3. Results
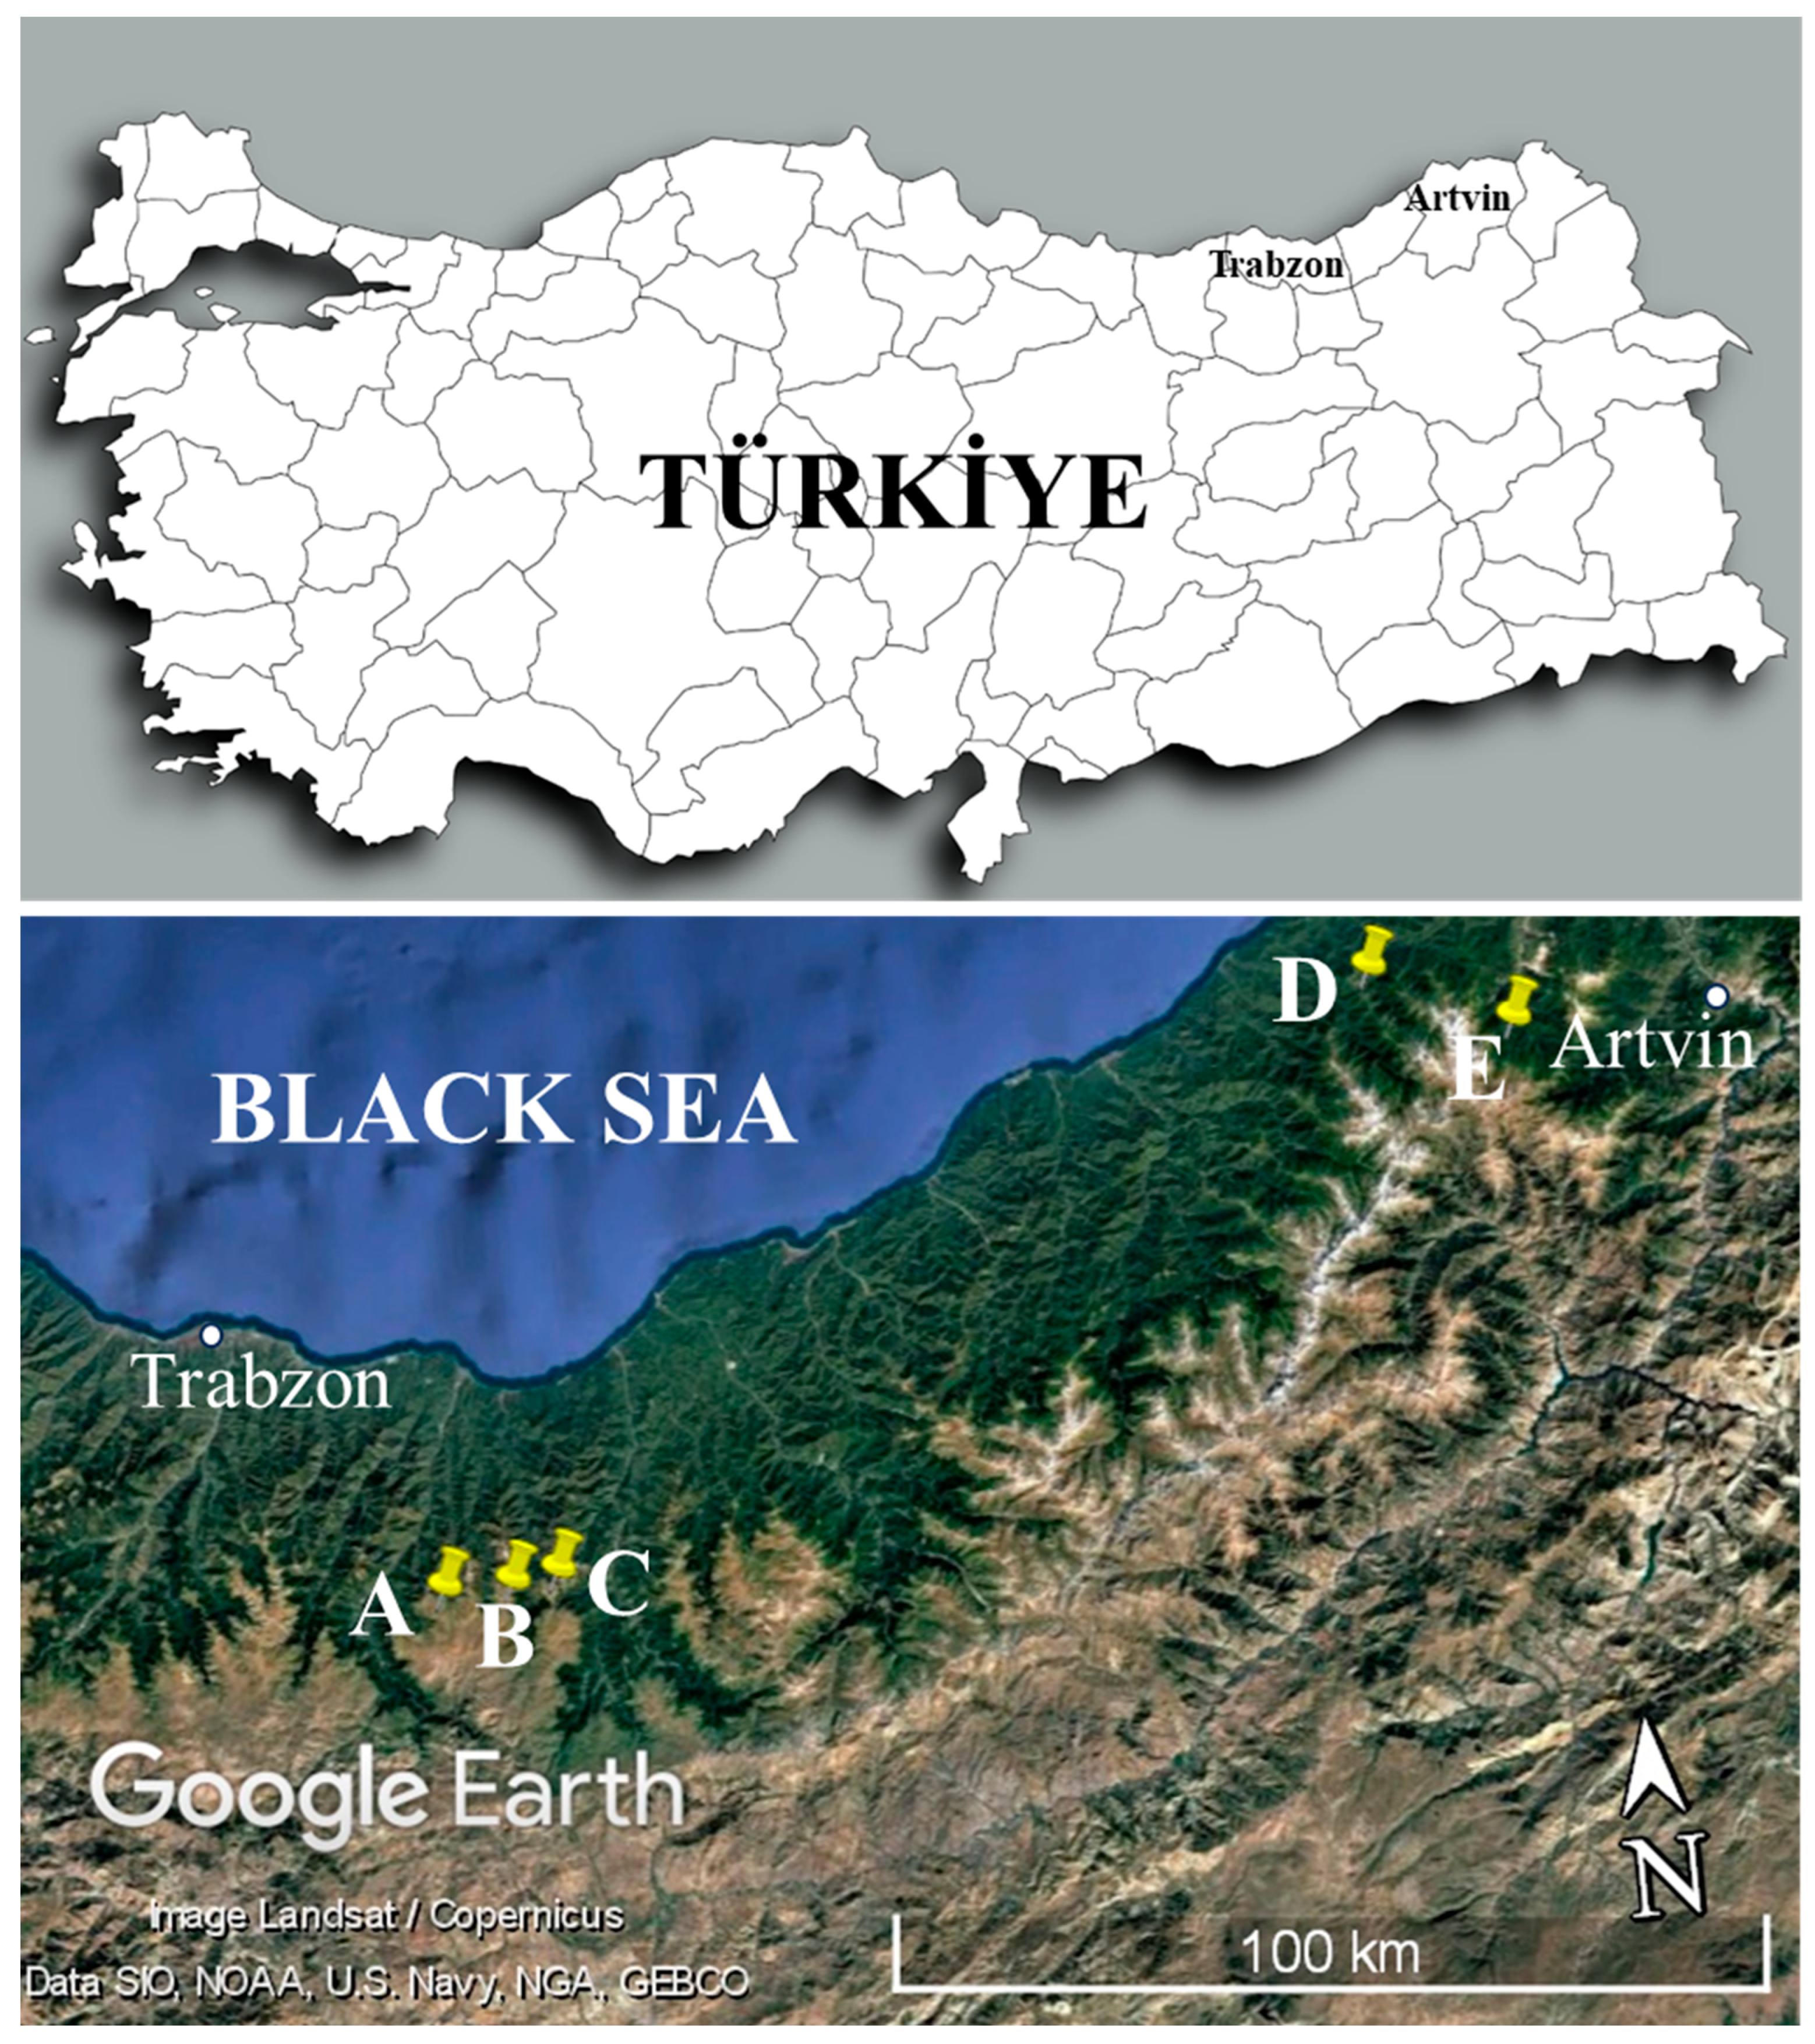
A total of 50 freshwater algal taxa belonging to 19 genera were identified as new records for the freshwater algal flora of Türkiye from the investigated blanket bog ecosystems. Among the taxa identified as new records, the algal assemblage was strongly dominated by Charophyta (desmids), while the remaining taxa belonged to Bacillariophyta, Cyanobacteriophyta, Chlorophyta, Euglenophyta, and Dinoflagellata, each represented by a limited number of species. Notably, the genera Calycimonas and Opisthoaulax were encountered for the first time in Türkiye, with their members recorded exclusively from the investigated blanket bog ecosystems.
Division: Cyanobacteriophyta
Genus: Scytonema C.Agardh ex Bornet and Flahault
Komárek [
49], p. 75, Figure 36.
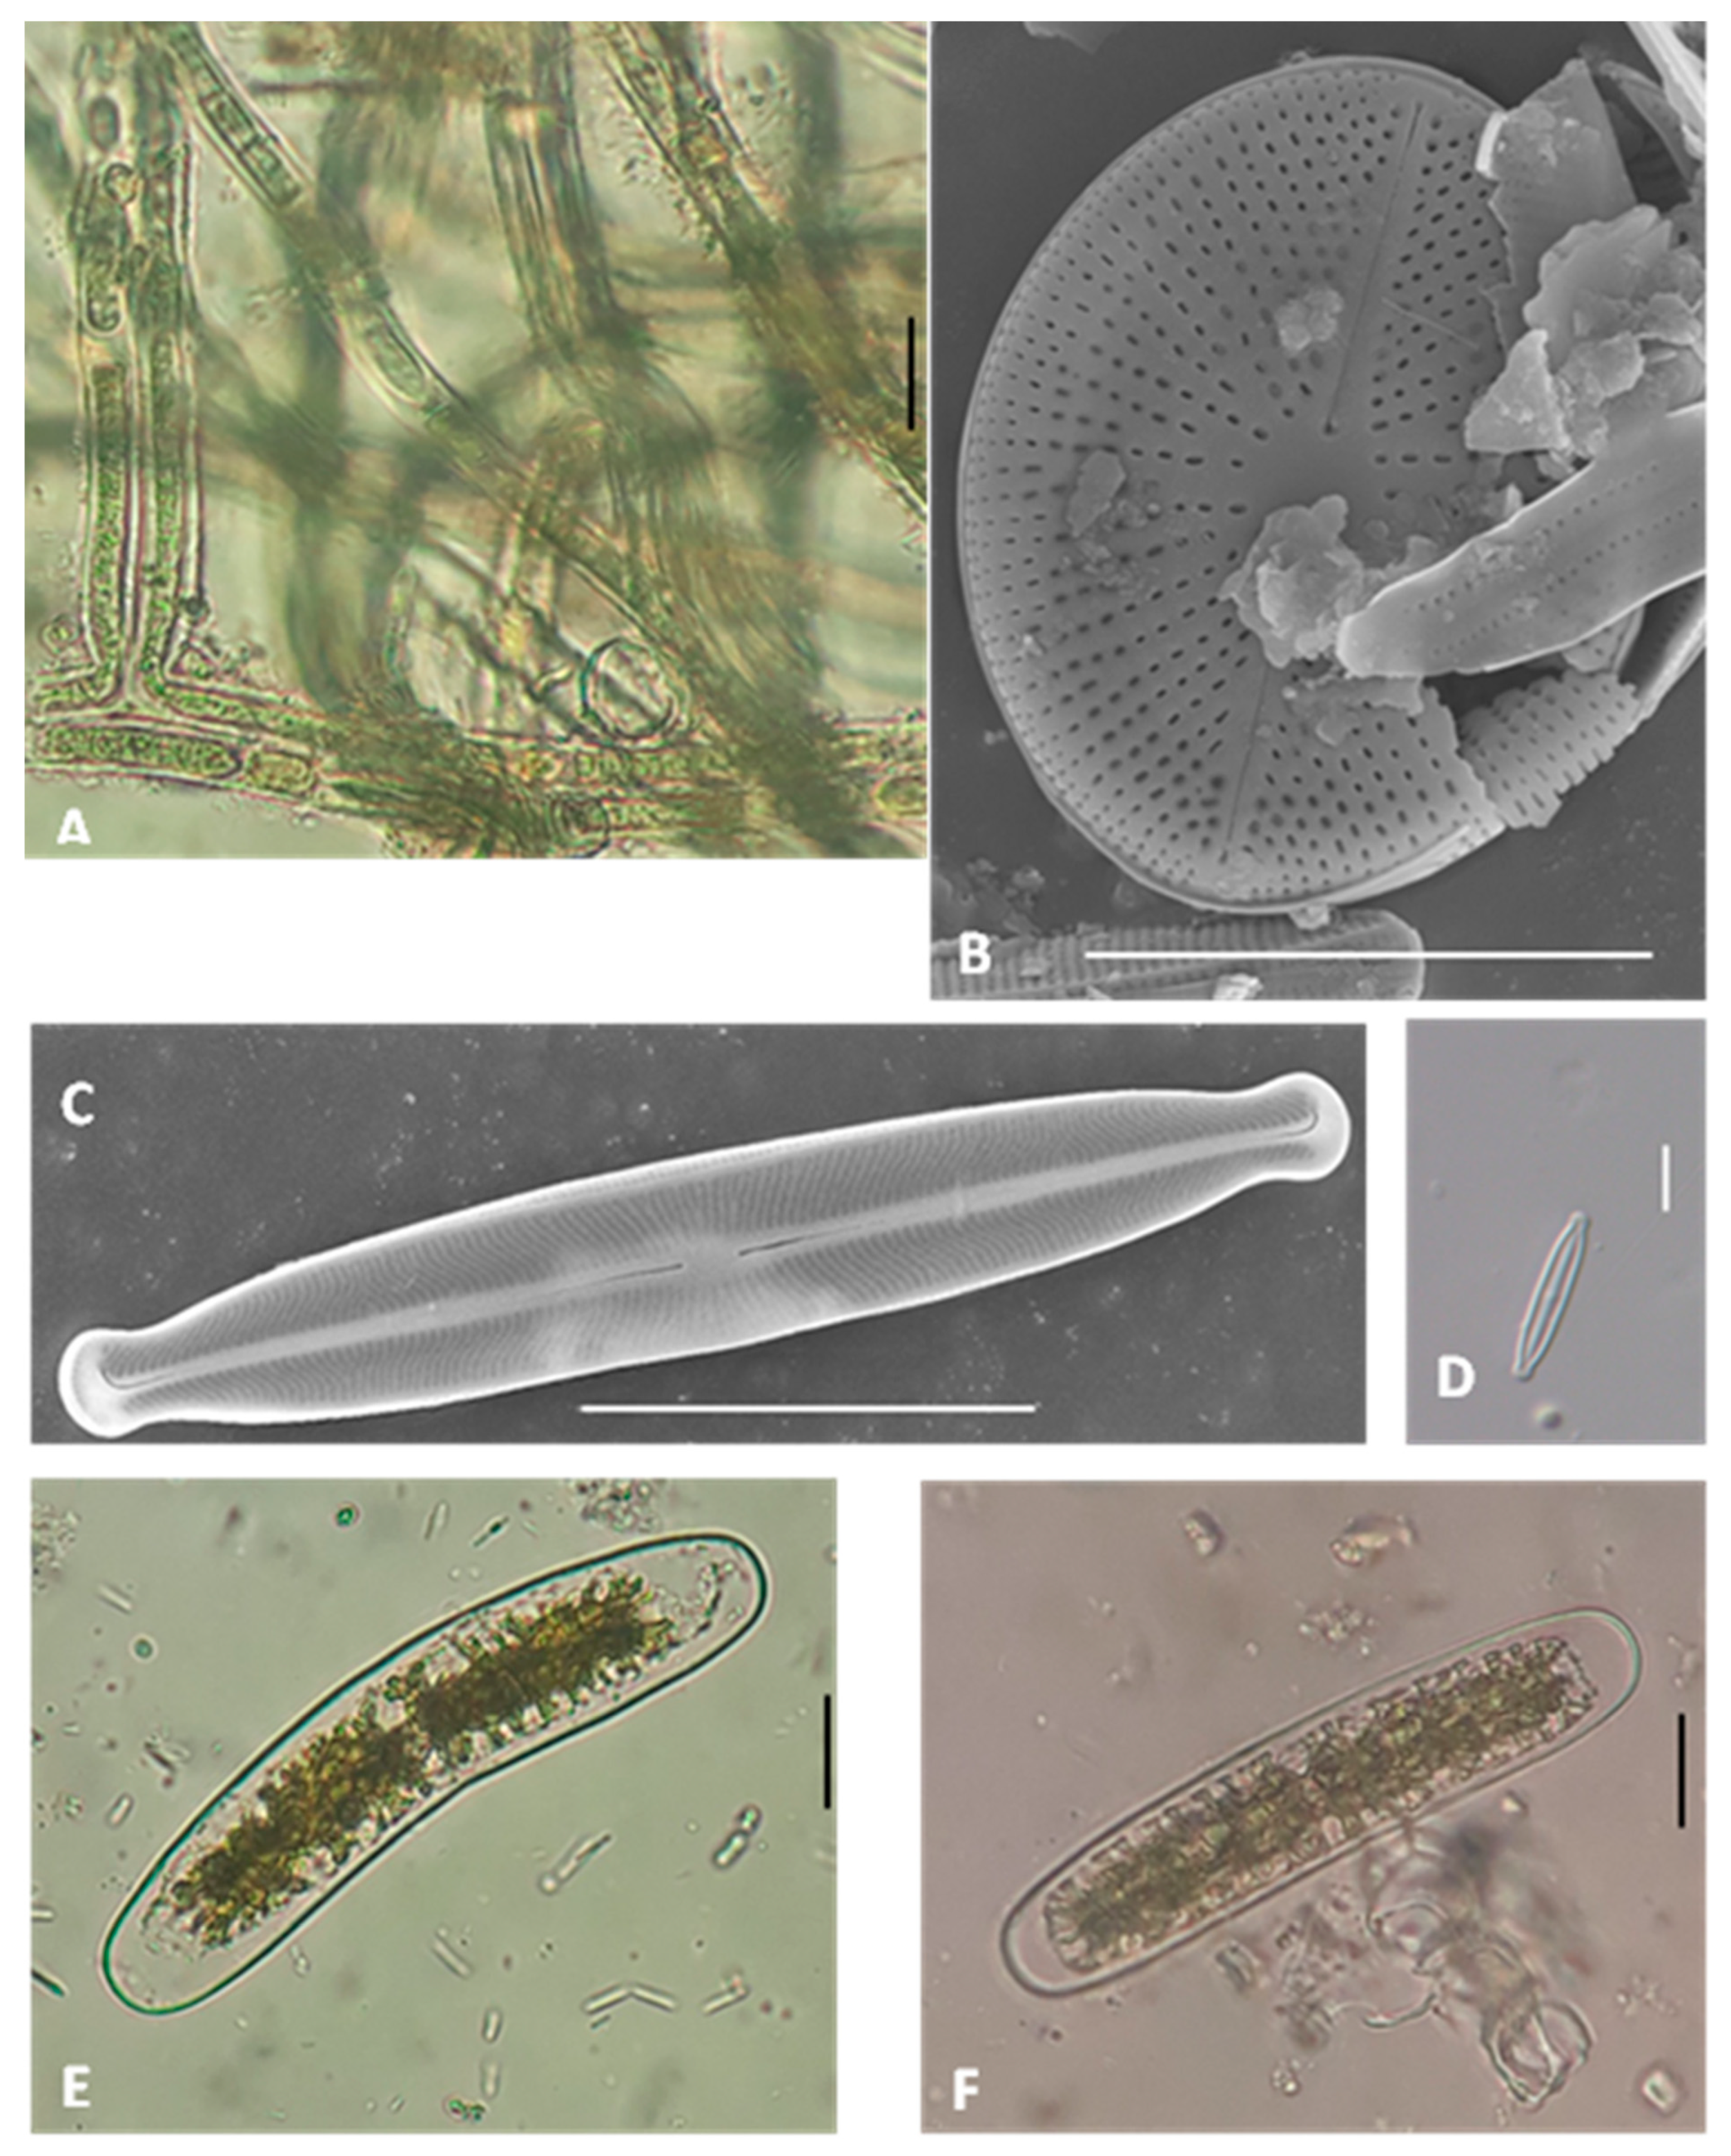
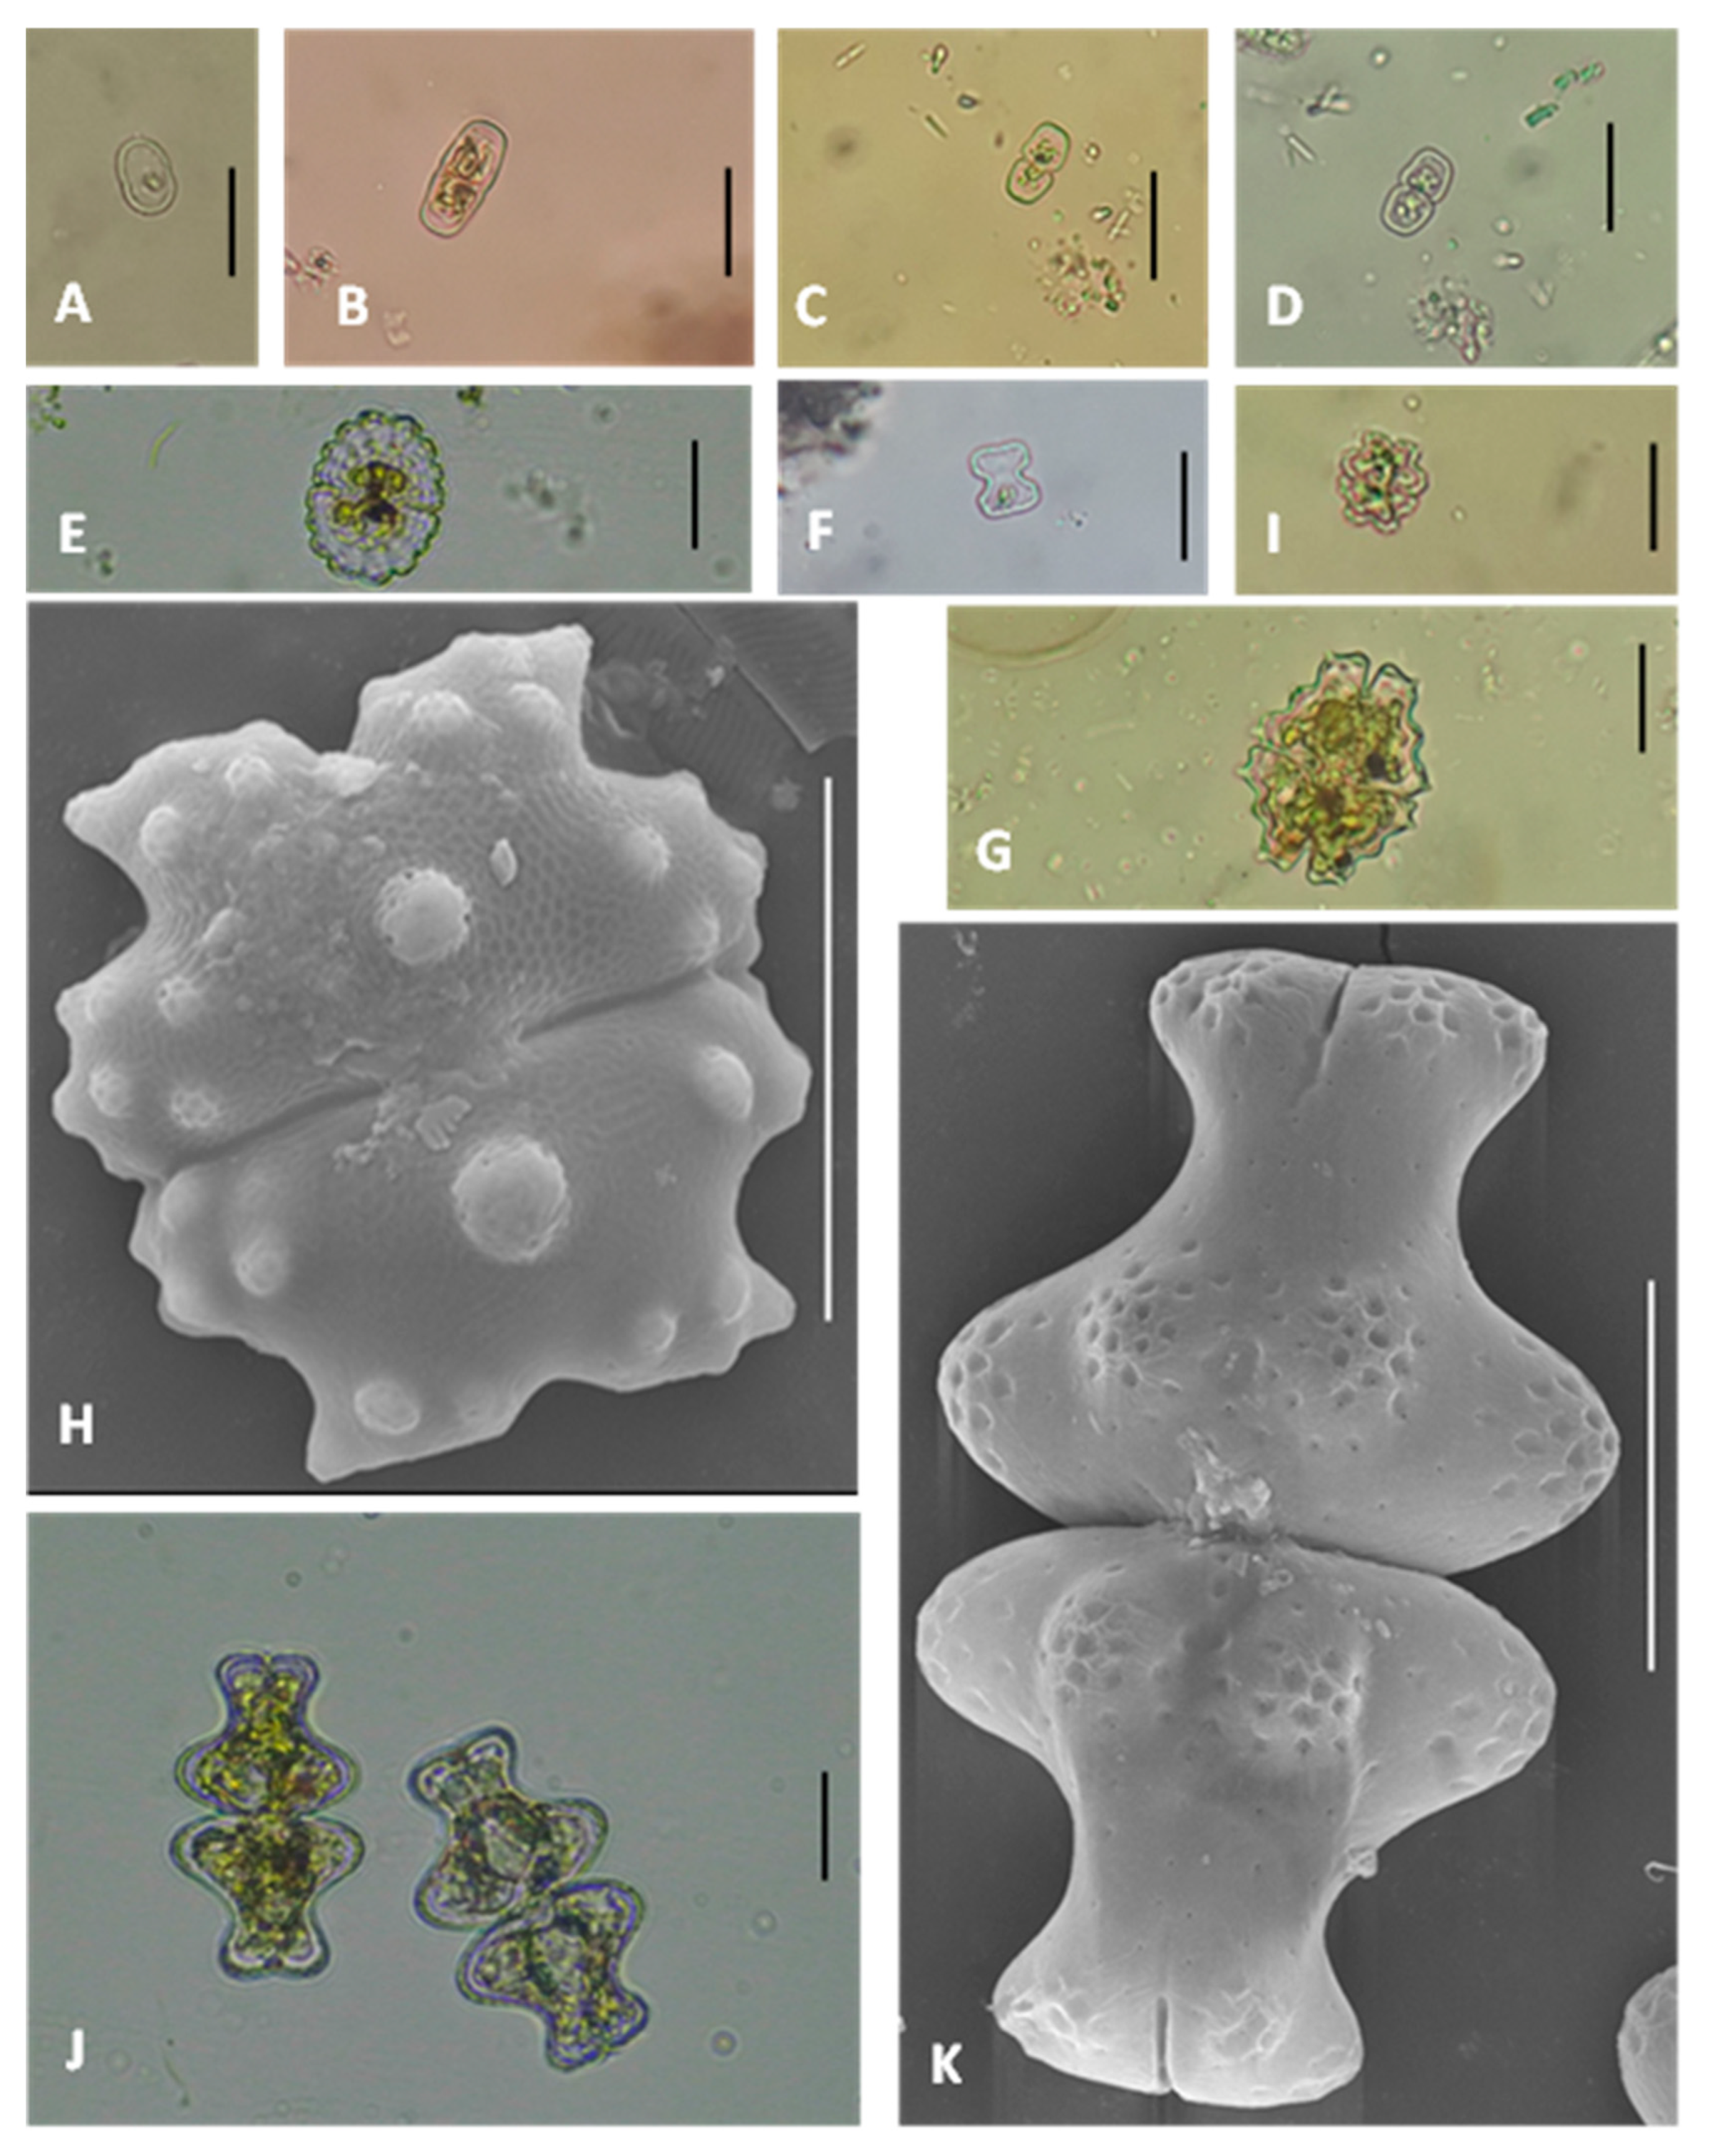
Description: Cells blue-green, cylindrical, slightly longer than wide (10 × 6 μm); filaments pseudo-branching (10 μm in diameter); heterocysts rectangular, 10 × 7 μm (
Figure 2A).
Habitat: The species was found as epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology: This taxon is widespread in stagnant waters, unpolluted lakes, ponds, acidic and soft water marshes, peat bogs. It is also widespread in wet soil [
49].
Division: Bacillariophyta
Genus: Cavinula D.G.Mann and Stickle
- 2.
Cavinula vincentii Antoniades and P.B.Hamilton 2009: 63, Figures 7–9, 12 and 13
Antoniades et al. [
44], p. 63, Figures 7–9, 12 and 13; Cvetkoska et al. [
50], p. 201, Figures 74–81, 172–180.
Description: Valves elliptical, with rounded ends. Size 15 × 2 μm (length × width). Striae 24/10 μm, strongly radiate, uniseriate; central area round, surrounded by long and short striae. Raphe filiform; areolae elliptical. An enlarged, transversely elongated pore-like fissure occurs near the distal ends on one side of the valve. This feature is characteristic of the species (
Figure 2B).
Habitat: The species was found in epipelic communities of bog pools in the Yılanlıtaş Blanket Bog.
Ecology: This species was first reported from a shallow, mineral-rich pond in the Canadian High Arctic [
44].
Genus: Kobayasiella Lange-Bertalot
- 3.
Kobayasiella parasubtilissima (H.Kobayasi and T.Nagumo) Lange-Bertalot 1999: 268
Alibert et al. [
51], p. 160, Figures 2A–P and 4A–H.
Description: Valves narrow and capitate at the ends, 28 × 4 μm; striae 48/10 μm; axial area linear; raphe linear with a slight median irregularity; central raphe fissures straight and well separated, terminal fissures gently curved opening outward (
Figure 2C,D).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in the Ağaçbaşı, Barma, Sazak, and Kabaca-Petek blanket bogs and with additional detection in the plankton of the Sazak Blanket Bog.
Ecology:
Kobayasiella parasubtilissima is a rare species typically associated with acidic, low-alkalinity lake environments [
51].
Division: Charophyta
Genus: Netrium (Nägeli) Itzigsohn and Rothe
- 4.
Netrium cylindricum (West and G.S.West) Coesel and Meesters 2023: 24, pl. 6: Figures 5 and 6
West and West [
19], p. 67, pl. 5, Figure 7; Förster [
29], p. 37, pl. 1, Figure 11; Brook and Williamson [
45], p. 57, pl. 22, Figures 1–19, pl. 23, Figures 1–8.
Description: Cell medium-sized, not constricted at the center. Free edges of chloroplasts with deep indentations. Cells strictly cylindrical; apices hemispherical. Slightly curved cells present within populations. The cell is 134 μm in length and 25 μm in breadth (
Figure 2E,F).
Habitat: It was found as atmophytic on Sphagnum in Barma and Kabaca-Petek blanket bogs.
Ecology: It is mainly found in boggy areas, especially on
Sphagnum in peatlands, and also occurs in the in littoral of acidic lakes [
19,
45].
- 5.
Netrium digitus var. lamellosum (Brébisson ex Kützing) Grönblad 1920: 13
Förster [
29], p. 35, pl. 1, Figure 8; Brook and Williamson [
45], p. 54, pl. 18, Figure 2.
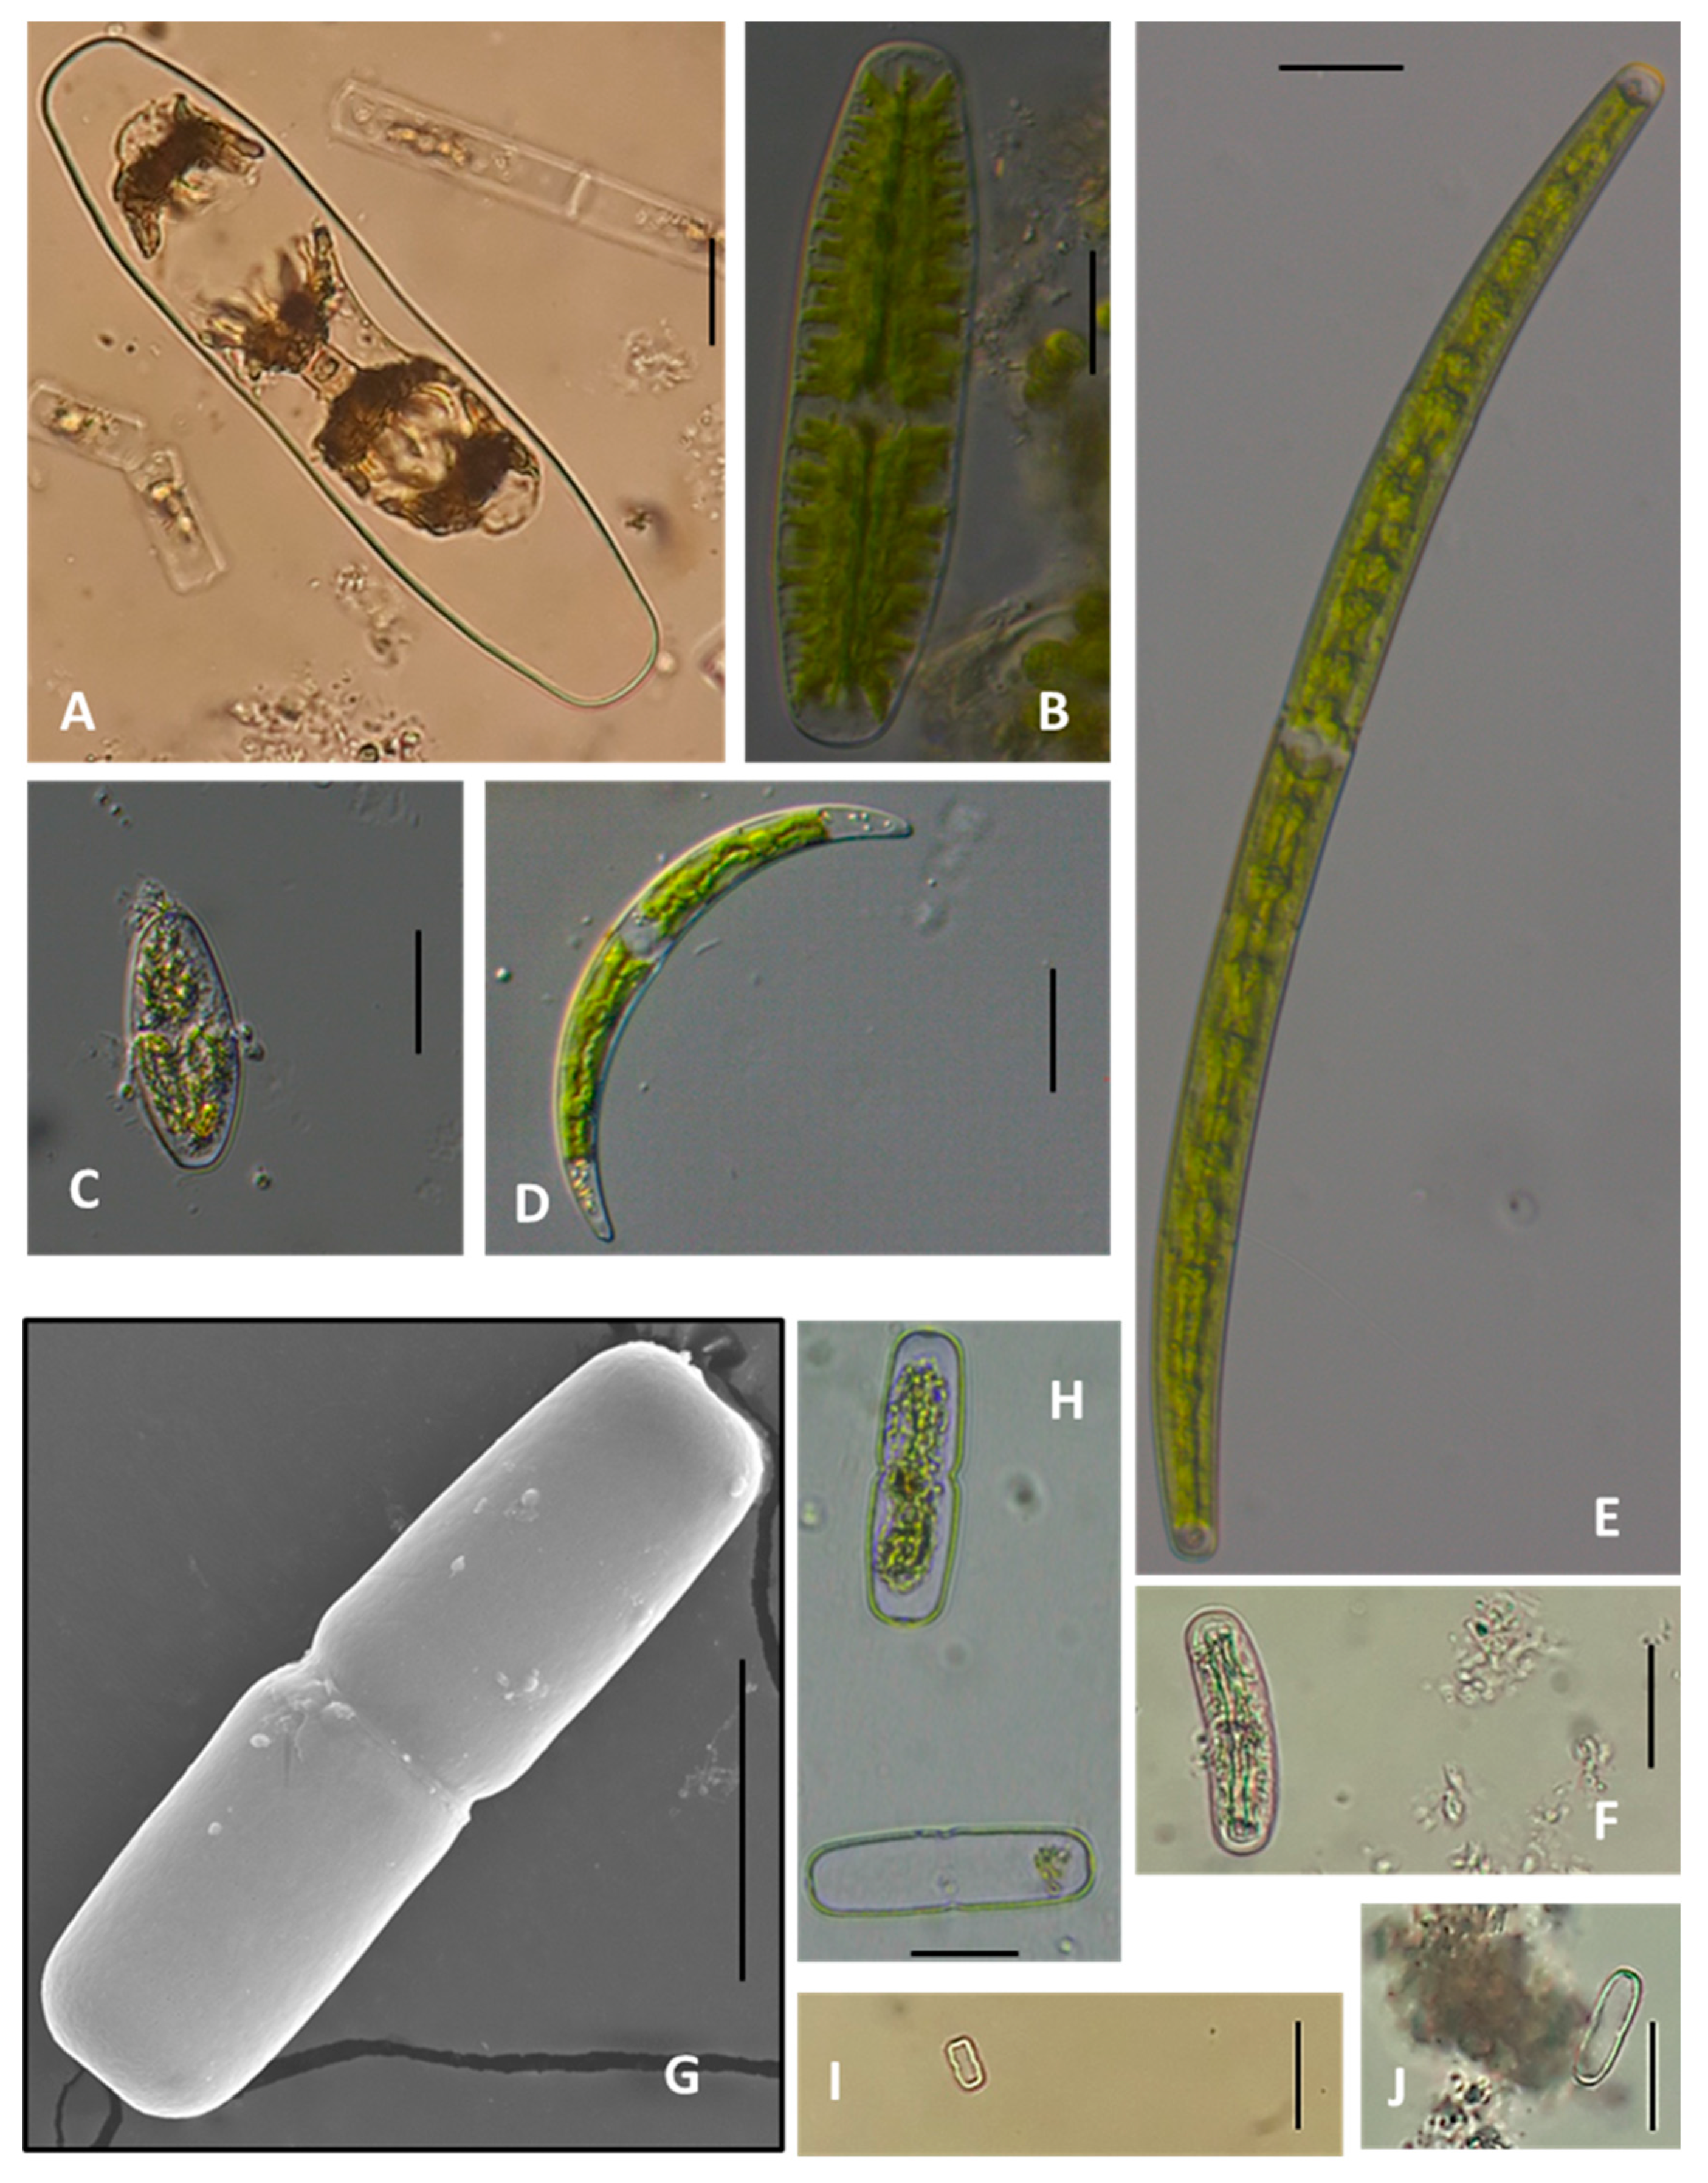
Description: Cells very slightly constricted at the center, with truncate and flattened apices; two axile chloroplasts each with four longitudinal ridges. The cell is 162 μm in length and 37 μm in breadth (
Figure 3A).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in the Ağaçbaşı Blanket Bog.
Ecology: The taxon is distributed as plankton and tychoplankton in acidic waters, particularly in littoral zone of lakes, ponds, and peat bogs, where the nominal variety is found. However, it is rare [
29,
45].
- 6.
Netrium naegelii (Brébisson ex W.Archer) West 1904: 66, pl. 7: Figures 4 and 5
West and West [
19], p. 66, pl. 7, Figures 4 and 5; Krieger [
25], p. 218, pl. 8, Figures 4 and 5; Förster [
29], p. 35, pl. 1, Figure 9; Brook and Williamson [
45], p. 55, pl. 20, Figures 1–8.
Description: Cells not narrowed in the midline; oblong–lanceolate; sharply rounded towards apex. Each semicell with a green axial chloroplast, edges bearing cut ridges. Similar to
Netrium digitus, but differs by smaller and narrower cells and chloroplast ridges number 5–6 in
Netrium digitus but only 1–2 in this taxon. The cell is 114 μm in length and 27 μm in breadth (
Figure 3B).
Habitat: The species was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in the Ağaçbaşı Blanket Bog.
Ecology: The taxon occurs in acidic to neutral stagnant waters, including puddles, ditches, marshes, and the littoral zones of oligotrophic and dystrophic ponds, and is also recorded as plankton in alpine lakes [
29].
- 7.
Netrium pseudactinotaenium Coesel 2002: 69, Figures 1–5, 12–14
Coesel and Meesters [
42], p. 23, pl. 4, Figures 1 and 2.
Description: Cell broadly fusiform–ellipsoid; apices round. Chloroplasts two, with longitudinal ridges. The cell is 40 μm in length and 17 μm in breadth, with a length-to-breadth ratio of 2.4 (
Figure 3C).
Habitat: The taxon was recorded in epipelic communities of bog pool in Barma Blanket Bog.
Ecology: It is oligotrophic [
42]. Its presence is limited to well-preserved biotopes that are almost unaffected by human activities [
11,
56].
Genus: Closterium Nitzsch ex Ralfs
- 8.
Closterium dianae var. minus Hieronymus 1895: 19, no figure
Coesel and Meesters [
42], p. 43, pl. 14, Figure 2; Brook and Williamson [
45], p. 285, pl. 134, Figure 5.
Description: Cells strongly curved, with the inner margin less curved than the outer; ventral side slightly swollen medially; apexes truncate with a small internal swelling (apical pore); stelloid chloroplasts with eight axile pyrenoids; cell wall smooth and colorless; cells smaller than the nominal variety. Cell length 86 μm, breadth 10 μm. Cells distinctly smaller than those of the nominal variety (180–300 × 20–30 μm), and the measured dimensions of the cell are 86 μm in length and 10 μm in breadth (
Figure 3D).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in the Ağaçbaşı Blanket Bog.
Ecology: It occurs in mesotrophic waters and is quite common in acidic habitats, especially moorland pools and fen hollows [
42,
45].
- 9.
Closterium directum W.Archer 1862: 249, pls. 12: Figures 23 and 24
Coesel and Meesters [
42], p. 43, pl. 25, Figures 1–3; Brook and Williamson [
45], p. 213, pl. 93, Figures 1–6.
Description: Cells slightly curved; sides parallel in mid region, attenuated middle to apex. Cell ends rarely recurved; apexes truncately rounded. Cell wall smooth. Stelloid chloroplasts with three longitudinal stripes; each containing eleven axillary pyrenoids. The cell is 258 μm in length and 14 μm in breadth (
Figure 3E).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma, Sazak and Kabaca-Petek blanket bogs.
Ecology: It is an acidophilic, cosmopolitan species commonly associated with
Sphagnum in acidic peat bogs [
42,
45]. Förster [
29] reported its occurrence as a tychoplankton in oligotrophic and mesotrophic lakes.
- 10.
Closterium pusillum Hantzsch 1861: no. 1008, Figures a–e
Kouwets [
34], p. 35, Figures 9–11; Coesel and Meesters [
42], p. 50, pl. 8, Figures 11–13; Brook and Williamson [
45], p. 240, pl. 108, Figures 1–15.
Description: Cell very slightly curved, slightly attenuated towards the ends. Lateral margins not strictly parallel, appearing nearly parallel in the midregion. Apex broadly rounded; colorless and smooth. Terminal vacuoles faintly visible at both apices. Two chloroplasts per cell, each with three longitudinal stripes; at least one pyrenoid per cell. The cell is 45 μm in length and 12 μm in breadth (
Figure 3F).
Habitat: The taxon was found as atmophytic on Sphagnum in Ağaçbaşı Blanket Bog.
Ecology: This species is commonly found in a semiatmophytic state on temporary water bodies and moist surfaces [
42]. Furthermore, detailed investigations have demonstrated the presence of the species in soil habitats as well [
57].
Genus: Actinotaenium (Nägeli) Teiling
- 11.
Actinotaenium crassiusculum (De Bary) Teiling 1954: 406, Figure 77
Lenzenweger [
37], p. 114, pl. 17, Figure 19; Kouwets [
34], p. 36, Figures 15–18; Coesel and Meesters [
42], p. 59, pl. 30, Figures 15–17.
Description: Cells cylindrical, apices truncately rounded; cell wall with irregularly distributed nanometer-sized pores. Chloroplast stelloid, the cell is 56 μm in length and 16 μm in breadth (
Figure 3G,H).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in the Sazak Blanket Bog and was also detected in the plankton of the Sazak Blanket Bog.
Ecology: It is characterized as acidophilic and oligotrophic, and is commonly found in strongly acidic
Sphagnum bogs at elevations up to 1700 m in the Alps [
37,
42]. Kouwets [
34] described
Actinotaenium crassiusculum as an arctic and alpine species occurring in acidic, oligotrophic environments.
- 12.
Actinotaenium geniculatum Kouwets 1988: 293, pl. I: Figures 10–15; pl. 6 [
33]
Kouwets [
33], p. 293, pl. 1, Figures 10–15, pl. 6, Figures 1 and 2.; Coesel and Meesters [
42], p. 61, pl. 31, Figures 31–37.
Description: Cells small, cylindrical; median constriction shallow. Lateral margins slightly undulate. Apices truncate–rounded; central region with slight indentation. Weakly geniculate. The cell is 9 μm in length and 5 μm in breadth. Species diminutive and inconspicuous, likely to be overlooked during routine microscopic examination (
Figure 3I).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology: It is found in acidophilic and oligotrophic regions [
33,
42,
58], and in moorland and bog pools [
42].
- 13.
Actinotaenium inconspicuum (West and G.S.West) Teiling 1954: 403, Figures 57 and 58
Lenzenweger [
37], p. 117, pl. 17, Figure 8; Coesel and Meesters [
42], p. 61, pl. 30, Figures 19 and 20.
Description: Cells small, narrow, cylindrical. Sides attenuate evenly towards apexes and truncate–rounded. Median constriction shallow. The cell is 21 μm in length, 7 μm in breadth (
Figure 3J).
Habitat: The species was recorded as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Kabaca-Petek Blanket Bog.
Ecology: It is rarely found in pools formed in bogs, and occurs in weakly acidic to neutral waters on moist rocks, and damp soil [
37,
42].
- 14.
Actinotaenium perminutum (G.S.West) Teiling 1954: 410, Figure 60
Coesel and Meesters [
42], p. 62, pl. 31, Figures 29 and 30; Szeląg-Wasielewska and Tomaszewicz [
41], p. 172, Figure 2.
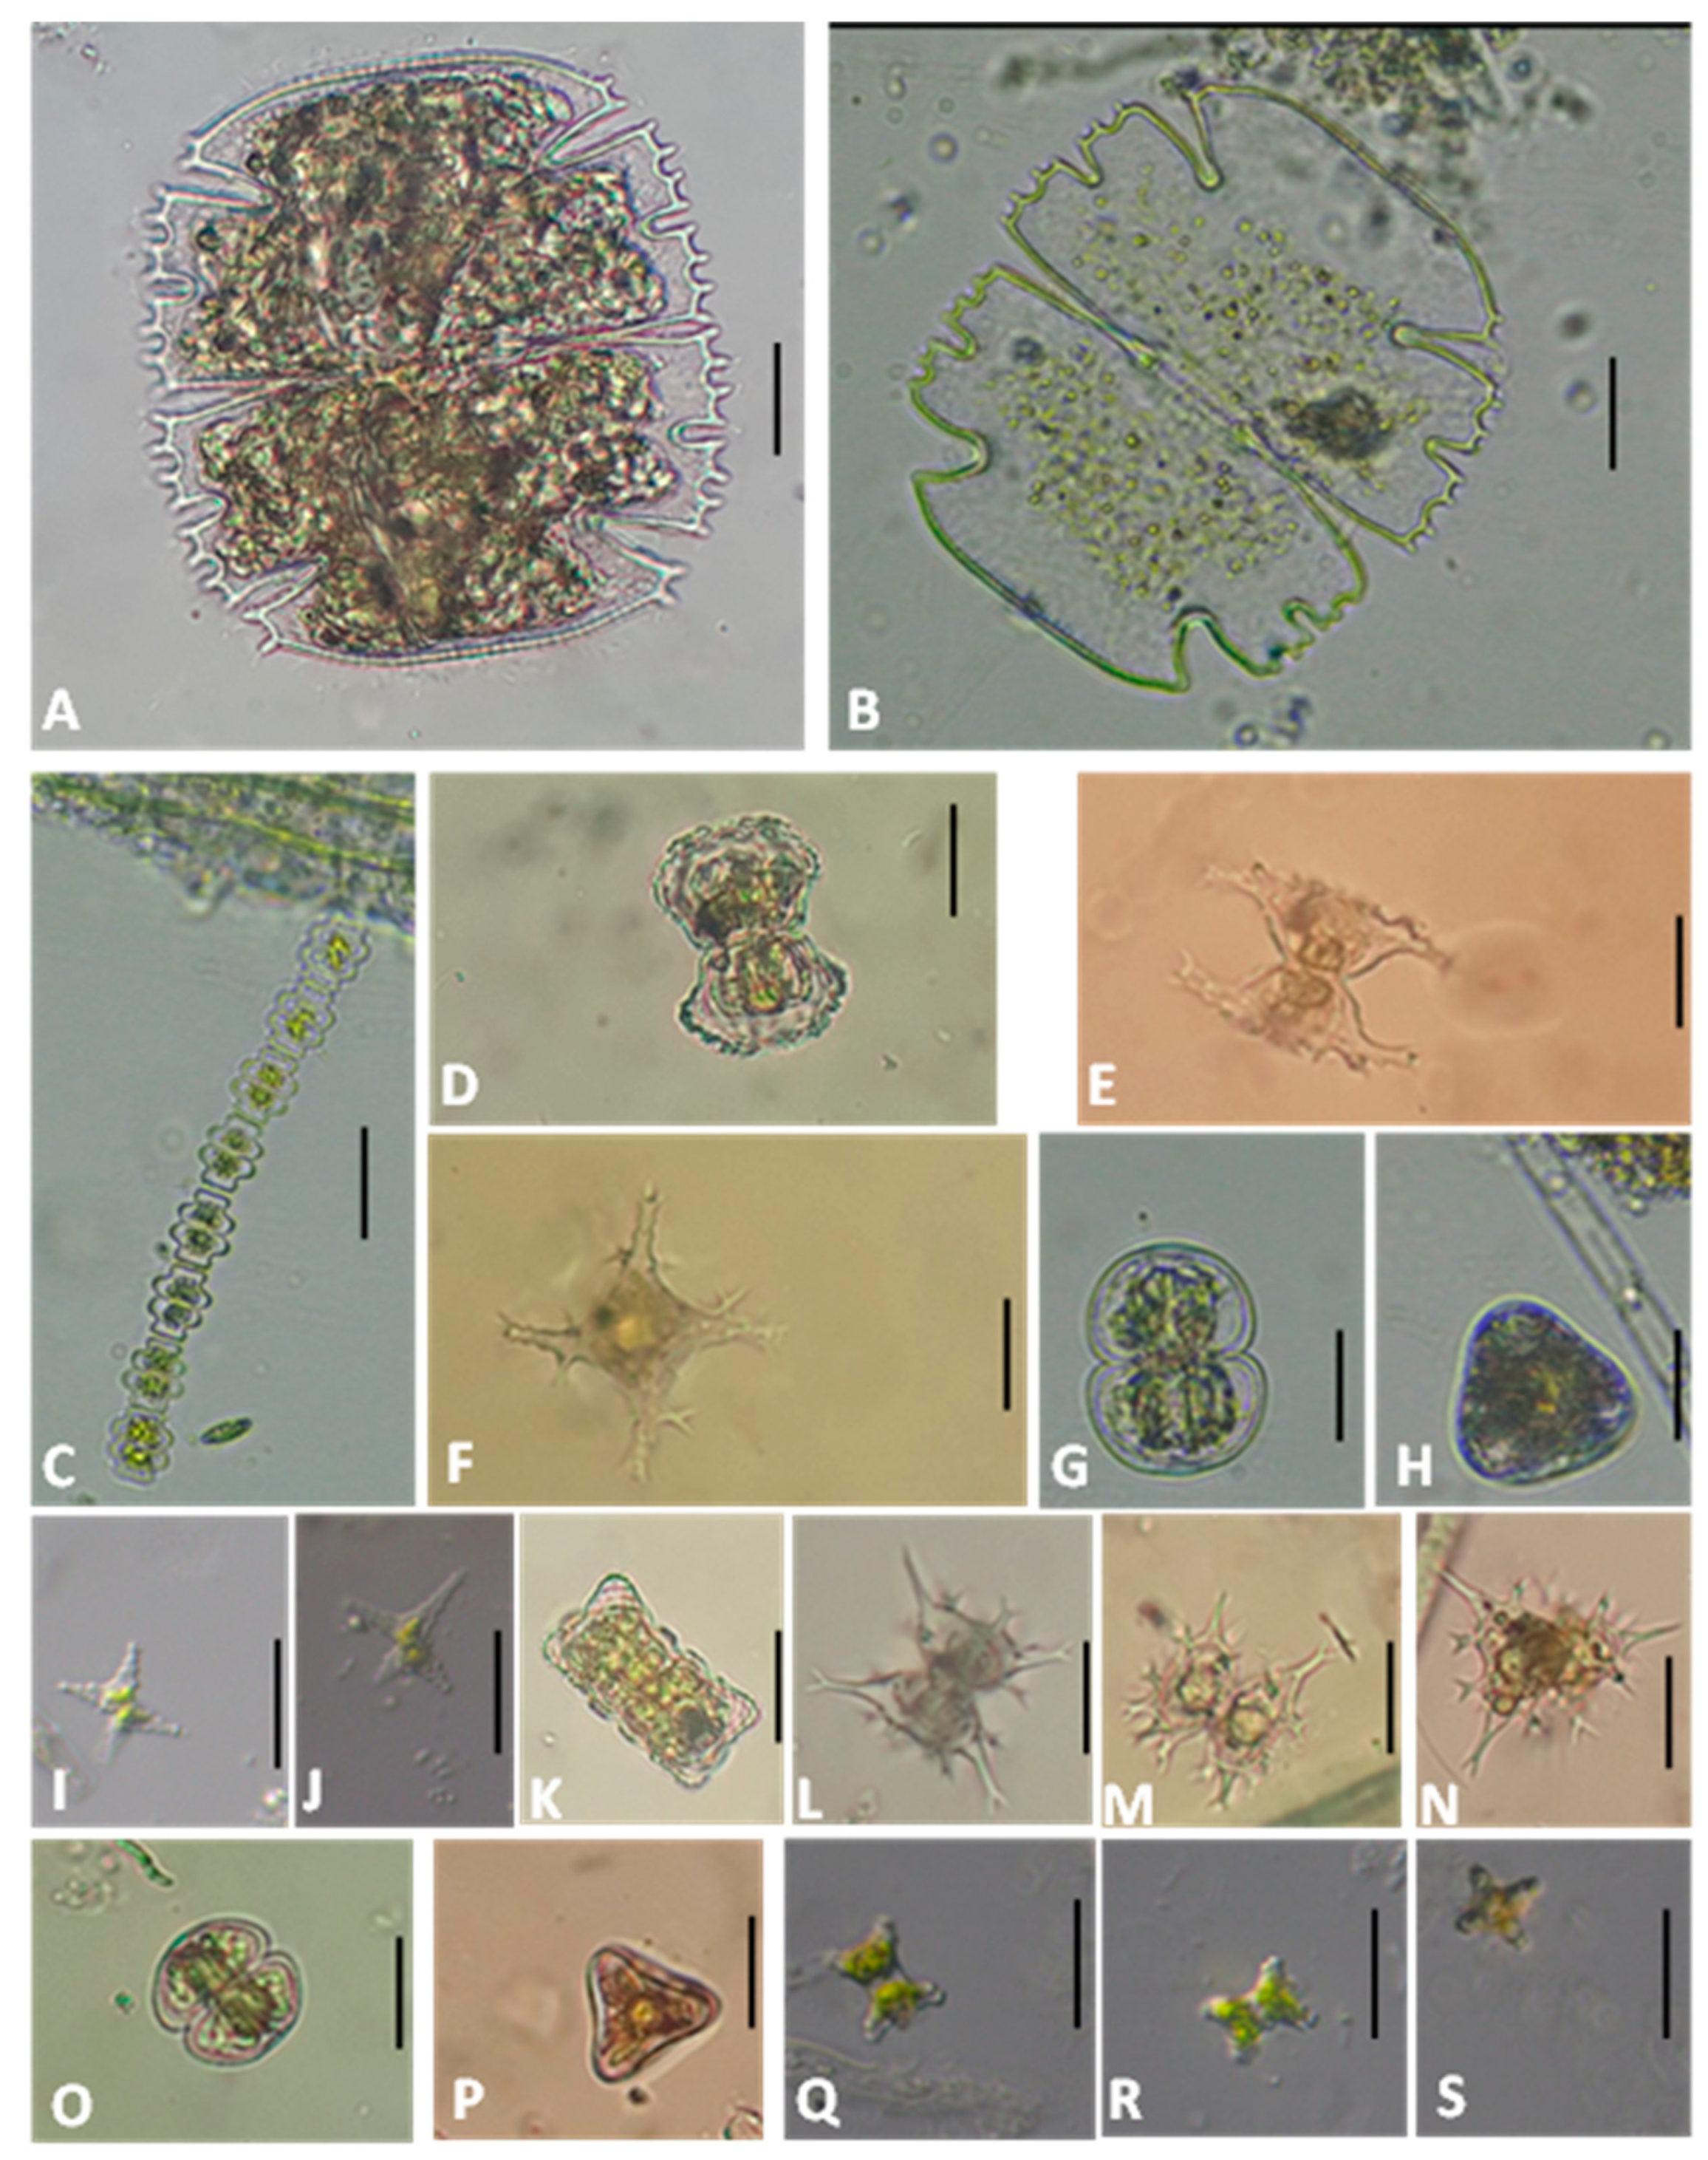
Description: Cells small; median constriction shallow with an open sinus. Semicells nearly globular, apices truncate–rounded. The cell is 14 μm in length, 8 μm in breadth (
Figure 4A).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog in Kabaca-Petek.
Ecology: An acidophilic and meso-oligotrophic species, it is frequently recorded on submerged
Sphagnum in bog pools [
41,
42].
- 15.
Actinotaenium pinicola Rosa 1959: 377, pls XX [
20]; XXI [
1]: Figure 1
Coesel and Meesters [
42], p. 63, pl. 31, Figure 16; Štěpánková et al. [
12], p. 117, Figure 4a; Mazalová et al. [
48], p. 10, pl. 1, Figure 22.
Description: Cells nearly cylindrical, with slightly truncate apices; lateral margins curved inward toward apex. Median constriction shallow. The cell is 23 μm in length and 9 μm in breadth (
Figure 4B).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology: This species is oligotrophic and acidophilic, and it also occurs in terrestrial environments [
42]. The species was recorded at all sites in the Jeseníky Mountains peatlands and is typical of subatmophytic microhabitats [
12]. It is abundant within
Sphagnum communities but rare in waters. Furthermore, Mazalová et al. [
48] documented this species in the flora of mesotrophic and oligo-mesotrophic peatlands.
Genus: Cosmarium Corda ex Ralfs
- 16.
Cosmarium anceps var. crispulum (Nordstedt) Willi Krieger and Gerloff 1965
Lenzenweger [
38], p. 75, pl. 51, Figure 27.
Description: Cells elongated; length nearly twice the breadth. Lateral margins converging toward apex. Semicells rounded trapezoidal; apex slightly concave. Isthmus broad; sinus shallow, narrow, notched. Lateral margins convex, differing from the nominate variety; basal and apical margins very slightly undulate. The cell is 17 μm in length and 8 μm in breadth (
Figure 4C,D).
Habitat: The taxon was recorded as epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in Kabaca-Petek Blanket Bog.
Ecology: The nominate variety is atmophytic and associated with arctic–alpine regions, occurring in humid continental zones above 2500 m, mainly among mosses on wet rocks or in stream splash zones, and rarely in slightly acidic mountain lake littoral zones [
38]. Information on var.
crispulum is scarce; it has been reported from the Austrian Alps and may share ecological preferences with the nominate variety [
38].
- 17.
Cosmarium nasutum Nordstedt 1872: 33, pl. VII [
7]: Figure 17
West and West [
21], p. 259, pl. 90, Figures 9 and 10.
Description: Cells small, elliptical, with a pronounced median constriction; sinus narrow and slightly expanded at the ends. Semicells semicircular; lateral margins convex and crenate, showing an apparent three-crenate pattern as a result of partial fusion of the basal crenation, although the underlying structure is four-crenate. Crenations bigranulate, not distinctly papillate. Apex shallowly retuse, with two apical crenations. Cell wall ornamented with granules arranged in radiating series, becoming less distinct toward the center. A slight central swelling is present above the isthmus. The cell is 32 μm in length and 25 μm in breadth; isthmus 12 μm (
Figure 4E).
Habitat: The taxon was found as epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology:
Cosmarium nasutum is a relatively rare desmid characteristic of alpine and arctic regions, occurring mainly in moist mountainous habitats, particularly in humid western areas [
21]. Within the species, forms such as f.
granulata have been reported from habitats including moss-covered rocks, wet soils, bogs, silt-covered slopes, and high-altitude ponds (>2200 m) [
38].
- 18.
Cosmarium truncatellum (Perty) Rabenhorst 1868: 165
Lenzenweger [
38], p. 72, pl. 51, Figure 18; Coesel and Meesters [
42], p. 148, pl. 60, Figure 31.
Description: Semicells rectangular with rounded angles; lateral margins slightly protruding; sinus deep and open. Apex broadly truncate, slightly concave; cell wall smooth. The cell is 13 μm in length and 11 μm in breadth (
Figure 4F).
Habitat: The species was found as epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Yılanlıtaş and Kabaca-Petek blanket bogs.
Ecology: It is acidophilic and oligotrophic [
42].
Genus: Euastrum Ehrenberg ex Ralfs
- 19.
Euastrum divaricatum P.Lundell 1871: 21, pl. II [
2]: Figure 5
West and West [
20], p. 42, pl. 38, Figures 3 and 4.; Förster [
29], p. 319, pl. 41, Figures 10 and 11; Lenzenweger [
37], p. 81, pl. 11, Figure 21; Coesel and Meesters [
42], p. 77, pl. 47, Figure 4.
Description: Semicells trapezoid; lobes broad, separated by inwardly curved incisions. Apex dome-shaped with a deep, narrow median incision; apical angles bearing small denticulations. Basal lobes rounded to truncate with spine-like processes. The cell is 43 μm in length and 33 μm in breadth (
Figure 4G).
Habitat: The taxon was observed as epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Sazak Blanket Bog.
Ecology: It is acidophilic, having been recorded in the wetlands at altitudes of 1700–2000 m in the Austrian Alps, particularly among
Sphagnum species [
37]. Additionally, it occurs in oligo- to mesotrophic aquatic habitats [
42].
- 20.
Euastrum gayanum De Toni 1889: 1075
Lenzenweger [
37], p. 81, pl. 11, Figure 9; Coesel and Meesters [
42], p. 78, pl. 47, Figures 22–25.
Description: Cells very small; semicells trapezoid, lacking lateral lobes. Apical lobes somewhat dilated toward apex; broad apices with a shallow V-shaped incision at mid-region. Small denticulations present along margins of apex. The cell is 14 μm in length and 14 μm in breadth; isthmus 3 μm (
Figure 4H,I).
Habitat: It was recorded as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology: It is acidophilic and mesotrophic [
42]. It is common in moorland pools and occurs up to a 2000 m altitude in the Alpine mountains [
37].
- 21.
Euastrum intermedium F.Gay 1884: 63
Lenzenweger [
37], p. 85, pl. 10, Figure 10; Coesel and Meesters [
42], p. 79, pl. 43, Figures 3 and 4.
Description: Semicells vase-shaped; neck region strongly constricted. Basal lobes broad and rounded; lateral lobes absent. Sinus margins convex and sinus sharply angled inward, widely open outward; Apices slightly anvil-shaped, with a deep, narrow median incision. The cell is 60 μm in length and 36 μm in breadth (
Figure 4J,K).
Habitat: It was recorded in epipelic communities, epiphytically on submerged plants in bog pools, and atmophytically on Sphagnum in Sazak Blanket Bog.
Ecology: The species is acidophilic and oligotrophic [
42] and is rare in moorland pools and has been recorded from acidic
Sphagnum-covered high-altitude bogs in the Alps at around 1700 m [
37].
Genus: Micrasterias C.Agardh ex Ralfs
- 22.
Micrasterias truncata var.
semiradiata Wolle 1884: pl. XXXVIII [
38]: Figure 7
Lenzenweger [
37], p. 109, pl. 14, Figure 4; Coesel and Meesters [
42], p. 91, pl. 51, Figure 7.
Description: Cells nearly circular; apex dome-shaped. Incisions between lobes more pronounced than in the nominate variety. Terminal lobes and apical angles clearly separated and dentate. The cell is 107 μm in length and 105 μm in breadth (
Figure 5A).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma, Yılanlıtaş, Sazak and Kabaca-Petek blanket bogs.
Ecology: The taxon is acidophilic and prefers oligo-mesotrophic conditions. It is commonly found in bogs and moorland pools, while it occurs only rarely in other types of habitats, particularly abundant in mesotrophic fen hollows [
42].
- 23.
Micrasterias truncata var. bahusiensis Wittrock 1869: 9, Figure 2
Lenzenweger [
37], p. 109, pl. 14, Figure 5; Coesel and Meesters [
42], p. 91, pl. 51, Figure 9.
Description: Cells roughly rectangular in outline. Apical lobes distinctly separated from upper lateral lobes by a wide incision. Angles of lobes prominent and dentate. The cell is 101 μm in length and 93 μm in breadth (
Figure 5B).
Habitat: The taxon was encountered as epipelic, epiphytic on submerged plants in bog pools in Kabaca-Petek Blanket Bog.
Ecology:
Micrasterias truncata var.
bahusiensis, described by Jan Šťastný [
11], is an oligo–mesotrophic, acidophilic benthic taxon considered rare in Czechia and rarely recorded from moorland pools [
42].
Genus: Spondylosium Brébisson ex Kützing
- 24.
Spondylosium pulchellum (W.Archer) W.Archer 1861: 72, pl. 3: Figure 104
West and West [
23], p. 227, pl. 161, Figures 1–3; Coesel and Meesters [
42], p. 206, pl. 119, Figures 18–21.
Description: Filamentous form, cells attached to substrates by means of a gelatinous basal stalk. Sinus deep, linear and closed, semicells truncate–pyramidal with concave sides, apex broad and flat, upper part sharp, almost rectangular in shape. Basal angles broadly rounded. The cell is 13 μm in length and 10 μm in breadth (
Figure 5C).
Habitat: The taxon was recorded as epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Sazak Blanket Bog.
Ecology: It is commonly found in oligotrophic and acidic bog pools [
42].
Genus: Staurastrum Meyen ex Ralfs
- 25.
Staurastrum bifasciatum Lütkemüller 1900: 77, pl. 1: Figures 43–47
Coesel and Meesters [
43], p. 72, pl. 58, Figures 15–18.
Description: Cells with campanulate semicells and a V-shaped sinus. Lateral sides concave; apices convex with slightly rounded apical corners and distinctly rounded lateral corners. Cell wall appearing verrucose and less distinct laterally on the median part of the cell. The cell is 41 μm in length and 30 μm in breadth (
Figure 5D).
Habitat: The species was found as epiphytic on submerged plants in bog pools in Barma Blanket Bog.
Ecology: It is a rarely encountered species, occurring in oligo-mesotrophic, acidic to neutral water bodies [
43].
- 26.
Staurastrum controversum var.
controversum Brébisson ex Ralfs 1848: 141, pl. XXIII [
23]: Figure 3a–g.
Coesel and Meesters [
42], p. 180, pl. 108, Figures 10–12; Coesel and Meesters [
43], p. 85, pl. 81, Figures 1–9.
Description: Semicells subelliptical, with distinctly convergent processes in frontal view; four processes visible in apical view, twisted in a clockwise direction. Cell wall ornamented with denticulations and spines of unequal size. Typically present dorsally at the base of each process is a pair of large, bifurcated spine-like structures. The cell is 28 μm in length and 47 μm in breadth (including the projections) (
Figure 5E,F).
Habitat: The taxon was reported as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Sazak Blanket Bogs.
Ecology:
Staurastrum controversum var.
controversum mainly inhabits benthic and tychoplanktonic habitats in acidic, oligotrophic freshwaters, while records from bogs and moorland pools are scarce [
42,
43].
- 27.
Staurastrum extensum (Nordstedt) Coesel and Meesters 2013: 95, pl. 33: Figures 17–19 [
43]
Coesel and Meesters [
43], p. 95, pl. 33, Figures 17–19.
Description: Sinus linear; cells with a deep median constriction. Semicells subelliptical, with broadly rounded angles; cell wall smooth. In apical view, cells triangular, with slightly concave margins and rounded angles. The cell is 40 μm in length and 33 μm in breadth (
Figure 5G,H).
Habitat: The taxon was collected as epipelic, epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology: It occurs in oligo- and mesotrophic water bodies [
43].
- 28.
Staurastrum minimum Coesel 1996: 23, Figures 20–23
Coesel and Meesters [
42], p. 190, pl. 115, Figures 11–14; Coesel and Meesters [
43], p. 121, pl. 91, Figures 4–7.
Description: Cells with a deep median constriction; sinus V-shaped. Semicells distinctly cup-shaped in outline, bearing three short, arm-like processes diverging from the apical region. Processes oriented in different planes. Processes with very small and faint denticulations, barely discernible under light microscopy. The cell is 19 μm in length and 17 μm in breadth (
Figure 5I,J).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Kabaca-Petek blanket bogs.
Ecology: It has only been recorded in certain acidic, oligotrophic moorland pools [
42,
43].
- 29.
Staurastrum pileolatum Brébisson 1848: 215, pl. XXXV [
35]: Figure 22
West and West [
22], p. 127, pl. 118, Figures 11–13; Coesel and Meesters [
43], p. 132, pl. 58, Figures 1–7.
Description: Cells with shallow sinus; semicells with distinctly concave lateral margins. Apices markedly flattened and nearly rectangular, with rounded corners. Apical wall bearing granules arranged in concentric series around angles. At base of semicells, a ring of granules present, separated from apical ornamentation by a clear zone. The cell is 36 μm in length and 20 μm in breadth (
Figure 5K).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in Ağaçbaşı, Barma, Yılanlıtaş and Kabaca-Petek blanket bogs.
Ecology:
Staurastrum pileolatum occurs in benthos of acidic, oligotrophic-to-mesotrophic water bodies such as bogs, mountain streams, and wetlands, particularly in the mountainous regions of Western and Central Europe [
22,
43].
- 30.
Staurastrum pseudopisciforme Eichler and Gutwiński 1894: 175, pl. V [
5]: Figure 50
Coesel and Meesters [
43], p. 137, pl. 120, Figures 7 and 8
Description: Constriction deep at middle; sinus open with acute angles. Semicells subelliptical, hexagonal, with lateral corners extended, divergent, and distinctly bifurcate. At apex, shorter similar projections present; a pair of smaller spines between each apical angle. In apical view, semicells three-radiate with straight arms. The cell is 33 μm in length and 41 μm in breadth (
Figure 5L–N).
Habitat: It was reported as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Sazak Blanket Bog.
Ecology: The species is distributed in acidic and nutrient-poor (oligotrophic) freshwater habitats [
43].
- 31.
Staurastrum ralfsii var.
depressum (J.Roy and Bisset) Coesel and Meesters 2013: 142, pl. 32: Figures 11–18 [
43].
Coesel and Meesters [
43], p. 142, pl. 32, Figures 11–18.
Description: Although in the nominal variety the cells are longer than broad, in var. depressum the cells about as broad as long. Semicells pyramidal and depressed; cell wall smooth. In apical view, semicells three-angled with broadly rounded corners and distinctly concave sides. The cell is 25 μm in length and 25 μm in breadth (
Figure 5O,P).
Habitat: The taxon was encountered as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma, Yılanlıtaş, Sazak and Kabaca-Petek blanket bogs.
Ecology: This species is found as both benthic and tychoplanktonic in oligo- to mesotrophic freshwater bodies with pH conditions ranging from acidic to neutral [
43].
- 32.
Staurastrum refractum Delponte 1877: 42, pl. XI [
11]: Figures 7–9
Coesel and Meesters [
42], p. 187, pl. 102, Figures 5 and 6; Coesel and Meesters [
43], p. 107, pl. 114, Figures 9–17.
Description: Most characteristic features of
Staurastrum refractum include small cell size, relatively wide and elongated isthmus, and four short arm-like processes constricted abruptly halfway along their length. Sinus broadly semicircular. Cells cup-shaped; in apical view, sides concave with four short arm-like projections. The cell is 16 μm in length and 14 μm in breadth (
Figure 5Q–S).
Habitat: It is recorded from epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology: The ecological characteristics associated with this species in earlier literature remain relevant under its current designation. It is acidophilic and oligotrophic [
43]. The observation by Homfeld [
59], noting that
S. refractum frequently occurs in old raised bog pools in the northwestern lowlands of Germany, was cited by Coesel and Hoogendijk [
60] as evidence of the species’ clear preference for oligotrophic–dystrophic environments. Additionally, it has been observed growing on
Sphagnum mosses in ditches and on aquatic vegetation along lake margins [
40].
- 33.
Staurastrum scabrum Brébisson 1848: 214, pl. XXXV [
35]: Figure 20
West and West [
23], p. 81, pl. 140, Figures 1 and 2; Coesel and Meesters [
42], p. 197, pl. 96, Figures 1–3; Coesel and Meesters [
43], p. 144, pl. 51, Figures 6–10.
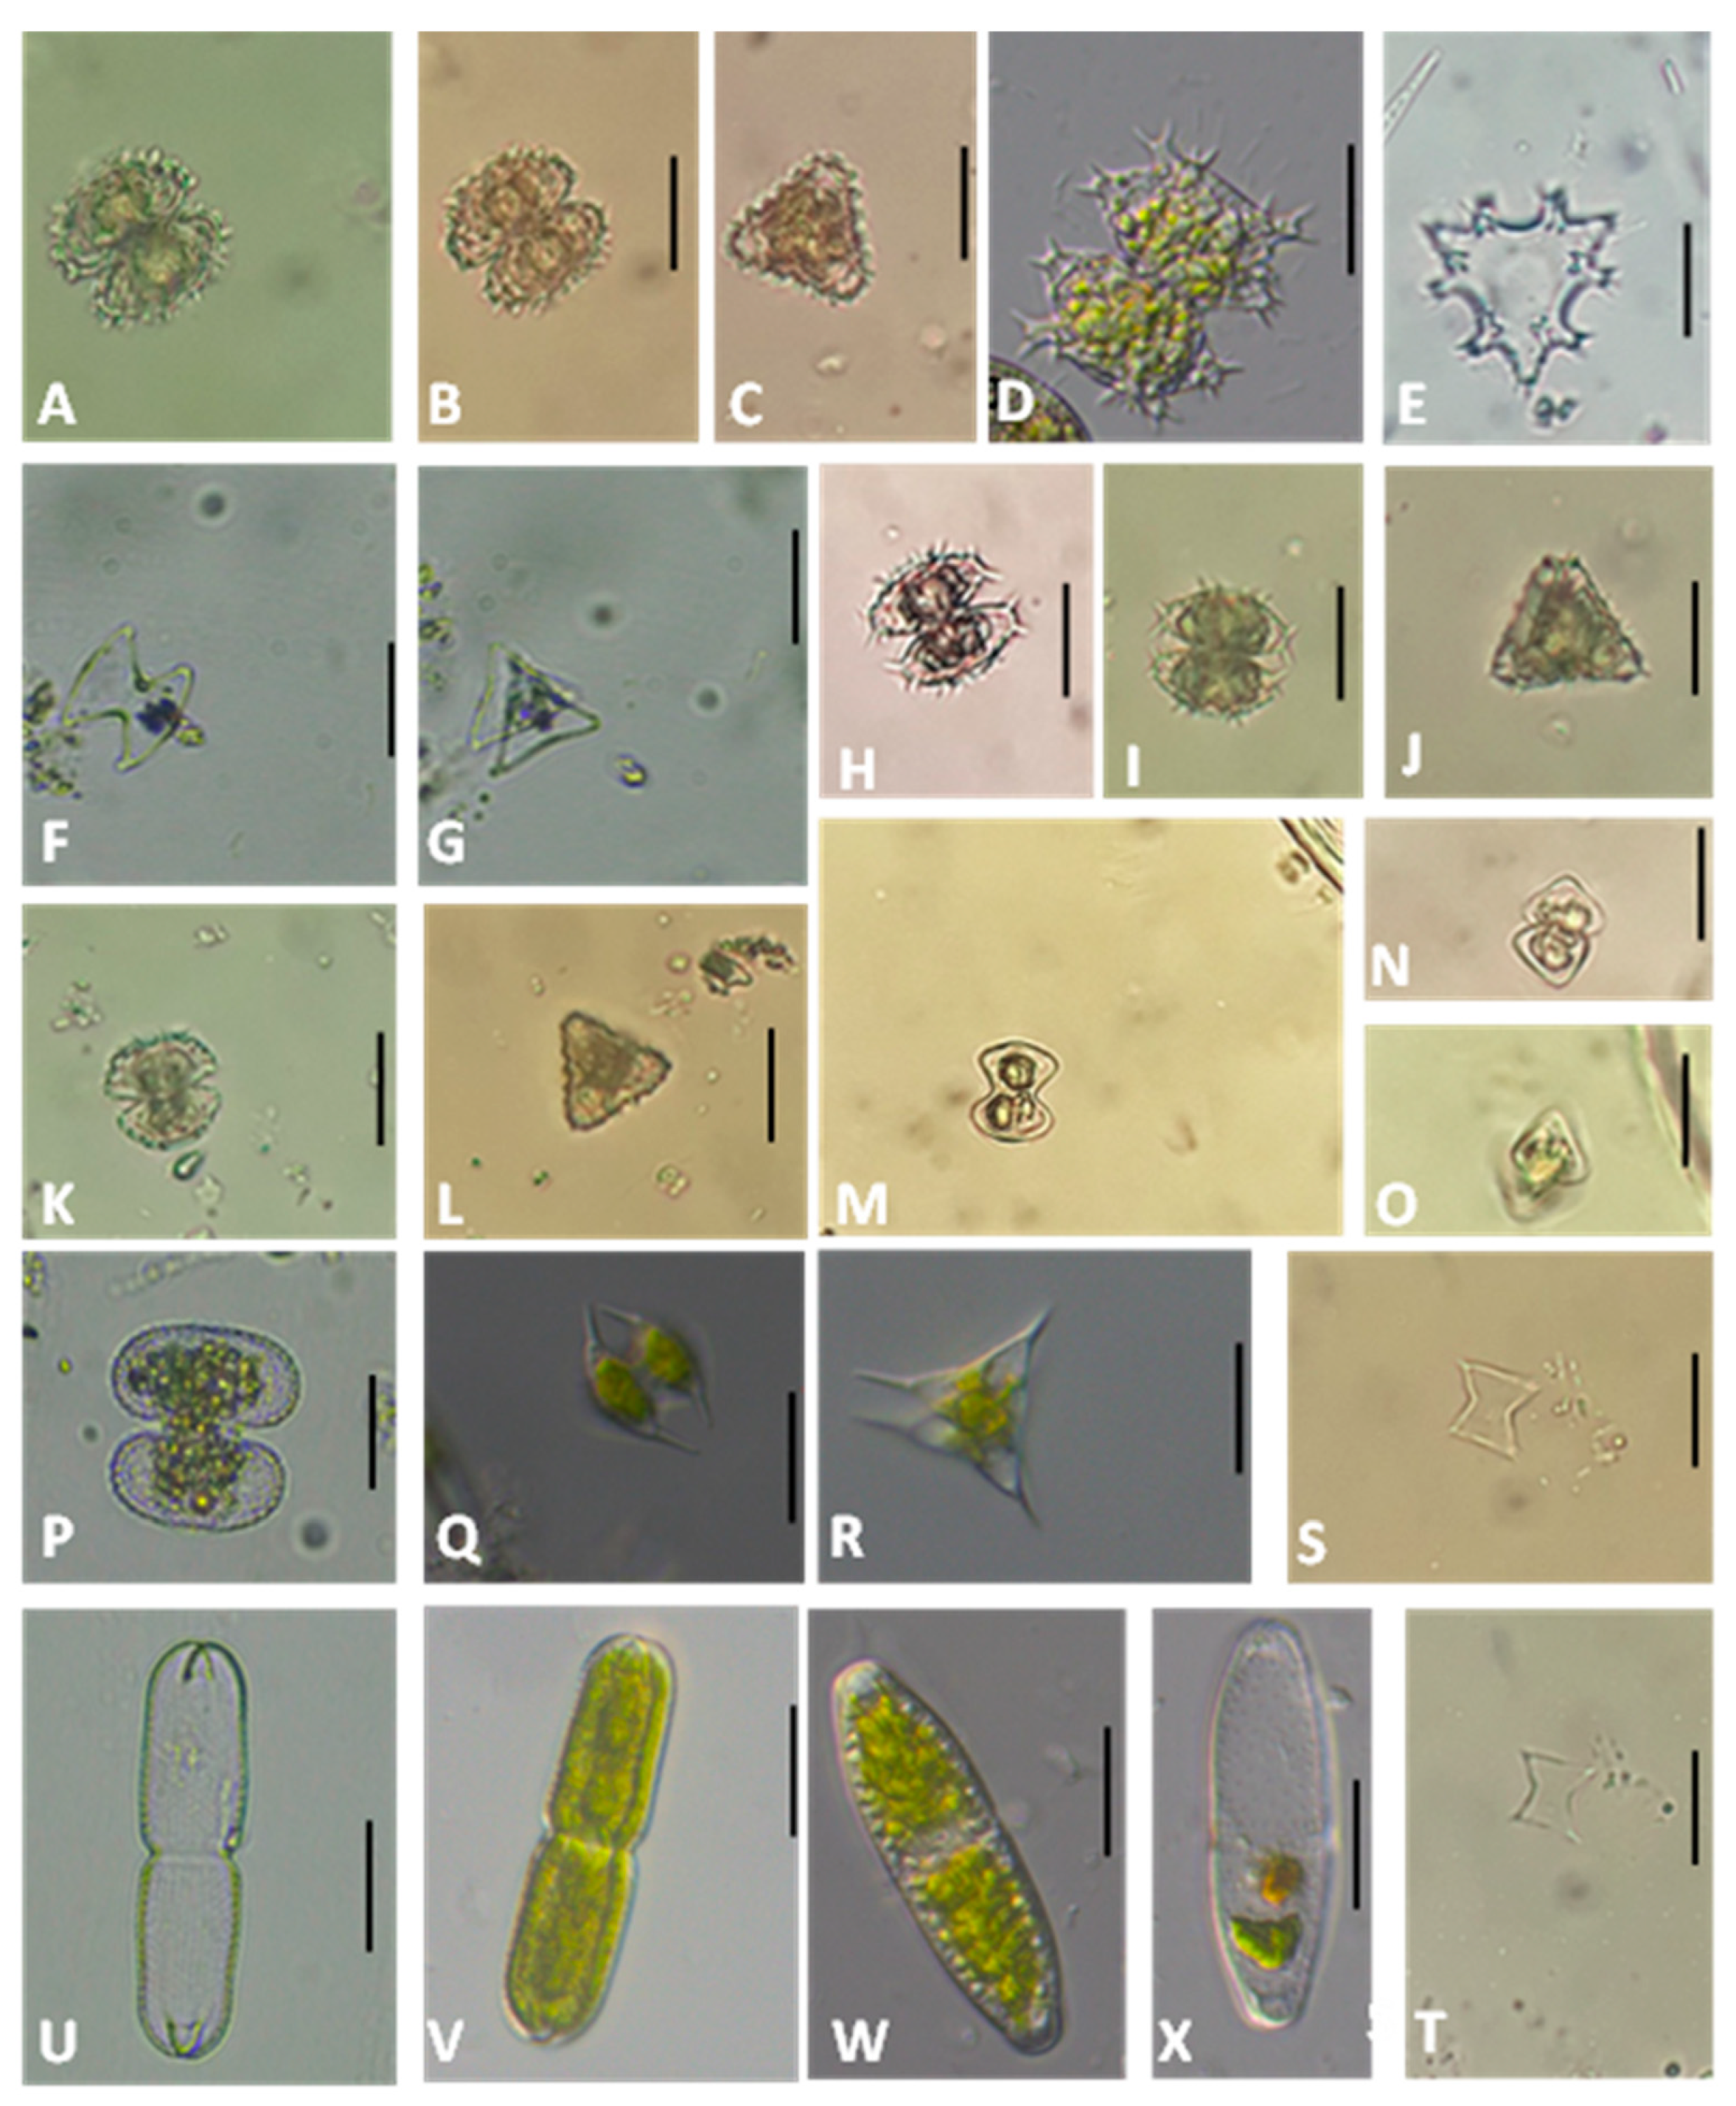
Description: Characterized by trapeziform semicells with broadly rounded basal angles. Cell wall bearing short spines arranged in concentric series around basal corners. Sinus open and acute. In apical view, cells three-angled with straight sides and rounded corners; rows of verrucae along margins and submarginal areas. The cell is 26 μm in length and 26 μm in breadth (
Figure 6A–C).
Habitat: The species was found as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in Ağaçbaşı, Yılanlıtaş, Sazak and Kabaca-Petek blanket bogs.
Ecology: It has been recorded from a wide range of locations across Europe and North America [
23]; primarily occurs in the benthic zone of oligotrophic and acidic freshwater bodies. In addition, it is relatively common in the arctic and alpine regions of Europe [
43].
- 34.
Staurastrum senarium Ralfs 1848: 216
West and West [
23], p. 175, pl. 156, Figure 3; Coesel and Meesters [
42], p. 197, pl. 98, Figures 10 and 11.
Description: Sinus open and acute and semicells elliptic, terminating at lateral angles in bifurcate, thickened surface projections formed in the same plane. Apical angles with prominent bifurcate processes. In apical view, cells triangular with slightly concave margins; two bifurcate processes arising from each side and two additional ones located just inside the apex of the upper margin. The cell is 45 μm in length and 39 μm in breadth (with spines) (
Figure 6D,E).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma and Yılanlıtaş blanket bogs.
Ecology:
Staurastrum senarium has been recorded in a mesotrophic peat bog pool of potential Holocene origin [
48]. Similarly, Coesel and Meesters [
43] indicated that the species is rare in mesotrophic hollows of Holocene fens.
- 35.
Staurastrum sibiricum O.Borge 1891: 9, Figure 4
Borge [
18], p. 9, Figure 4; West and West [
22], p. 152, pl. 122, Figures 17–19; Coesel and Meesters [
43], p. 148, pl. 26, Figures 11–15.
Description: Semicells subtriangular with narrowly acute apical angles, each bearing a distinct thickening at the apex. Cell wall smooth. In apical view, cells appear triangular with distinctly narrow apical corners. The cell is 19 μm in length and 21 μm in breadth (
Figure 6F,G).
Habitat: It was observed as epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology: This species is found in both planktonic and benthic communities of acidic, oligotrophic waters, and has also been observed growing subatmophytic on dripping rock surfaces [
43].
- 36.
Staurastrum simonyi var.
simonyi Heimerl 1891: 67, pl. V [
5]: Figure 23.
Coesel and Meesters [
42], p. 198, pl. 96, Figures 4–6; Coesel and Meesters [
43], p. 149, pl. 62, Figures 7–12.
Description: Cells elliptic in shape. Sinus open and acute. Two spine-like projections extending from lateral corners in the same vertical plane. Four well-developed spine-like processes present on apical margins. In apical view, cells exhibiting three or four acute angles. The cell is 22 μm in length and 27 μm in breadth (
Figure 6H–J).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma, Sazak and Kabaca-Petek blanket bogs.
Ecology: It is acidophilic and oligotrophic, and it occurs only rarely in bog habitats [
42].
- 37.
Staurastrum simonyi var. semicirculare Coesel 1996: 25, Figures 27 and 28
Coesel and Meesters [
42], p. 198, pl. 96, Figures 7–10; Coesel and Meesters [
43], p. 149, pl. 62, Figures 17–20.
Description: Cells slightly longer than broad, with a deep median constriction and an open sinus. Semicells semicircular. Four spines on apical angles; a series of spines at basal angles. The cell is 20 μm in length and 20 μm in breadth (
Figure 6K,L).
Habitat: It was recorded as epipelic and epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology: The taxon prefers oligotrophic and acidic waters [
11,
43]. Štěpánková et al. [
61] reported that
Staurastrum simonyi var.
semicirculare was found in several peat bogs in Czechia, occurring in acidic waters.
- 38.
Staurastrum thomassonii Nygaard 1991: 213, pl. 4: Figures 79–81; pl. 7: Figure 120a,b
Nygaard [
35], p. 213, pl. 4, Figures 79–81; pl. 7, Figure 12a–b; Coesel and Meesters [
43], p. 159, pl. 34, Figures 7–11.
Description: Cells triradiate in apical view, slightly longer than broad. Semicells subpyramidal with rounded apices in frontal view [
35]. Sinus widely open, acute-angled to nearly rectangular. Isthmus broad, exceeding half of the cell breadth. Cell wall smooth. In apical view, cells subtriangular with broadly rounded angles; sides straight to slightly concave. The cell is 18 μm in length and 14 μm in breadth (L/B = 1.3), isthmus 8 μm (
Figure 6M–O).
Habitat: It was found as epipelic and atmophytic on Sphagnum in Ağaçbaşı Blanket Bogs.
Ecology: The taxon has been reported from an oligotrophic lake in Denmark, where it occurred in low numbers during the summer months (May–October) and was not recorded in winter [
35].
- 39.
Staurastrum turgescens De Notaris 1867: 51, pl. IV [
4]: Figure 43
Coesel and Meesters [
43], p. 162, pl. 53, Figures 1–4.
Description: Sinus open and acute; cells deeply constricted. Apex narrow and rounded. Semicells elliptic–oval. Cell wall granulates, with densely arranged granules. Cells slightly longer than broad. The cell is 36 μm in length and 34 μm in breadth (
Figure 6P).
Habitat: The species was observed as epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology:
Staurastrum turgescens occurs as benthic and tychoplanktonic in acidic and oligo-mesotrophic water bodies, and exhibits a cosmopolitan distribution across Europe [
43].
Genus: Staurodesmus
- 40.
Staurodesmus glaber var. debaryanus (Nordstedt) Teiling 1967: 558, pl. 14: Figures 2 and 3
Coesel and Meesters [
42], p. 162, pl. 87, Figures 20 and 21.
Description: Cells with a deep median constriction and an open sinus. Semicells triangular, with convergent spines (7 μm long) at apical angles. Variety characterized by convex apices, differing from others. The cell is 18 μm in length and 16 μm in breadth (excluding spines) (
Figure 6Q,R).
Habitat: The taxon was encountered as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı, Barma and Yılanlıtaş blanket bogs.
Ecology: It is found in moorland pools and prefers oligo-mesotrophic and acidic conditions [
42].
- 41.
Staurodesmus omearae (W.Archer) Teiling 1948: 254, pl. XXI [
21]: Figures 8–13
Coesel and Meesters [
43], p. 32, pl. 14, Figures 5–22.
Description: Sinus widely open; semicells cup-shaped, with short divergent spines at apical angles. The cell is 14 μm in length and 15 μm in breadth (including spines) (
Figure 6S,T).
Habitat: It was reported as epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in Kabaca-Petek Blanket Bog.
Ecology: This species is cosmopolitan and exhibits a wide distribution across Europe, where it is frequently found in high abundances [
43].
Genus: Tetmemorus Ralfs ex Ralfs
- 42.
Tetmemorus brebissonii var.
minor De Bary 1858: 73, Figure 9; pl. V [
5]
Förster [
29], p. 299, pl. 39, Figure 11; Kouwets [
32], p. 212, pl. 5, Figures 6 and 7; Lenzenweger [
37], p. 63, pl. 8, Figure 12; Coesel and Meesters [
42], p. 70, pl. 39, Figure 6.
Description: Cells slightly compressed, cylindrical in frontal view; lateral sides straight and parallel, narrowed slightly towards ends. Apices broadly rounded with closed apical depression. Longitudinal striae visible on cell wall, discernible only in absence of chloroplasts. Variety characterized by smaller dimensions compared to nominal variety (length 55–100 μm). The cell is 74 μm in length and 18 μm in breadth (
Figure 6U,V).
Habitat: The taxon was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in Ağaçbaşı and Barma blanket bogs.
Ecology: It frequently occurs in bogs and moorland pools, and can be present in substantial quantities both in lowland regions and at higher elevations, such as the Alps up to 2000 m above sea level [
37,
42,
61,
62].
- 43.
Tetmemorus laevis var. minutus (De Bary) Willi Krieger 1937: 457, pl. 55: Figures 8 and 9
Coesel and Meesters [
42], p. 70, pl. 39, Figure 3.
Description:
Tetmemorus laevis Ralfs ex Ralfs 1848 is roughly similar to
T. granulatus Brébisson ex Ralfs, which is characterized by fusiform cells and scattered cell wall pores. In frontal view, cells narrowing moderately from central region toward ends; lateral sides convex at mid-region, becoming concave near apices. Apices relatively broadly rounded, with distinct deep median inward fold. Cells of
T. laevis generally smaller and less narrowed toward ends compared to
T. granulatus. In addition, var.
minutus distinguished by even smaller cells. The cell is 69 μm in length and 19 μm in breadth (
Figure 6W,X).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in the Ağaçbaşı, Barma, Sazak, and Kabaca-Petek blanket bogs. It has also been detected in the plankton of Sazak Blanket Bog.
Ecology: The taxon is acidophilic and oligotrophic. It occurs subatmophytically on
Sphagnum mosses and on wet soil [
42].
Division: Chlorophyta
Genus: Microspora Thuret
- 44.
Microspora pachyderma (Wille) Lagerheim 1887: 415
Prescott [
28], p. 108, pl. 8, Figure 3; John et al. [
40], p. 453, Figure 116J.
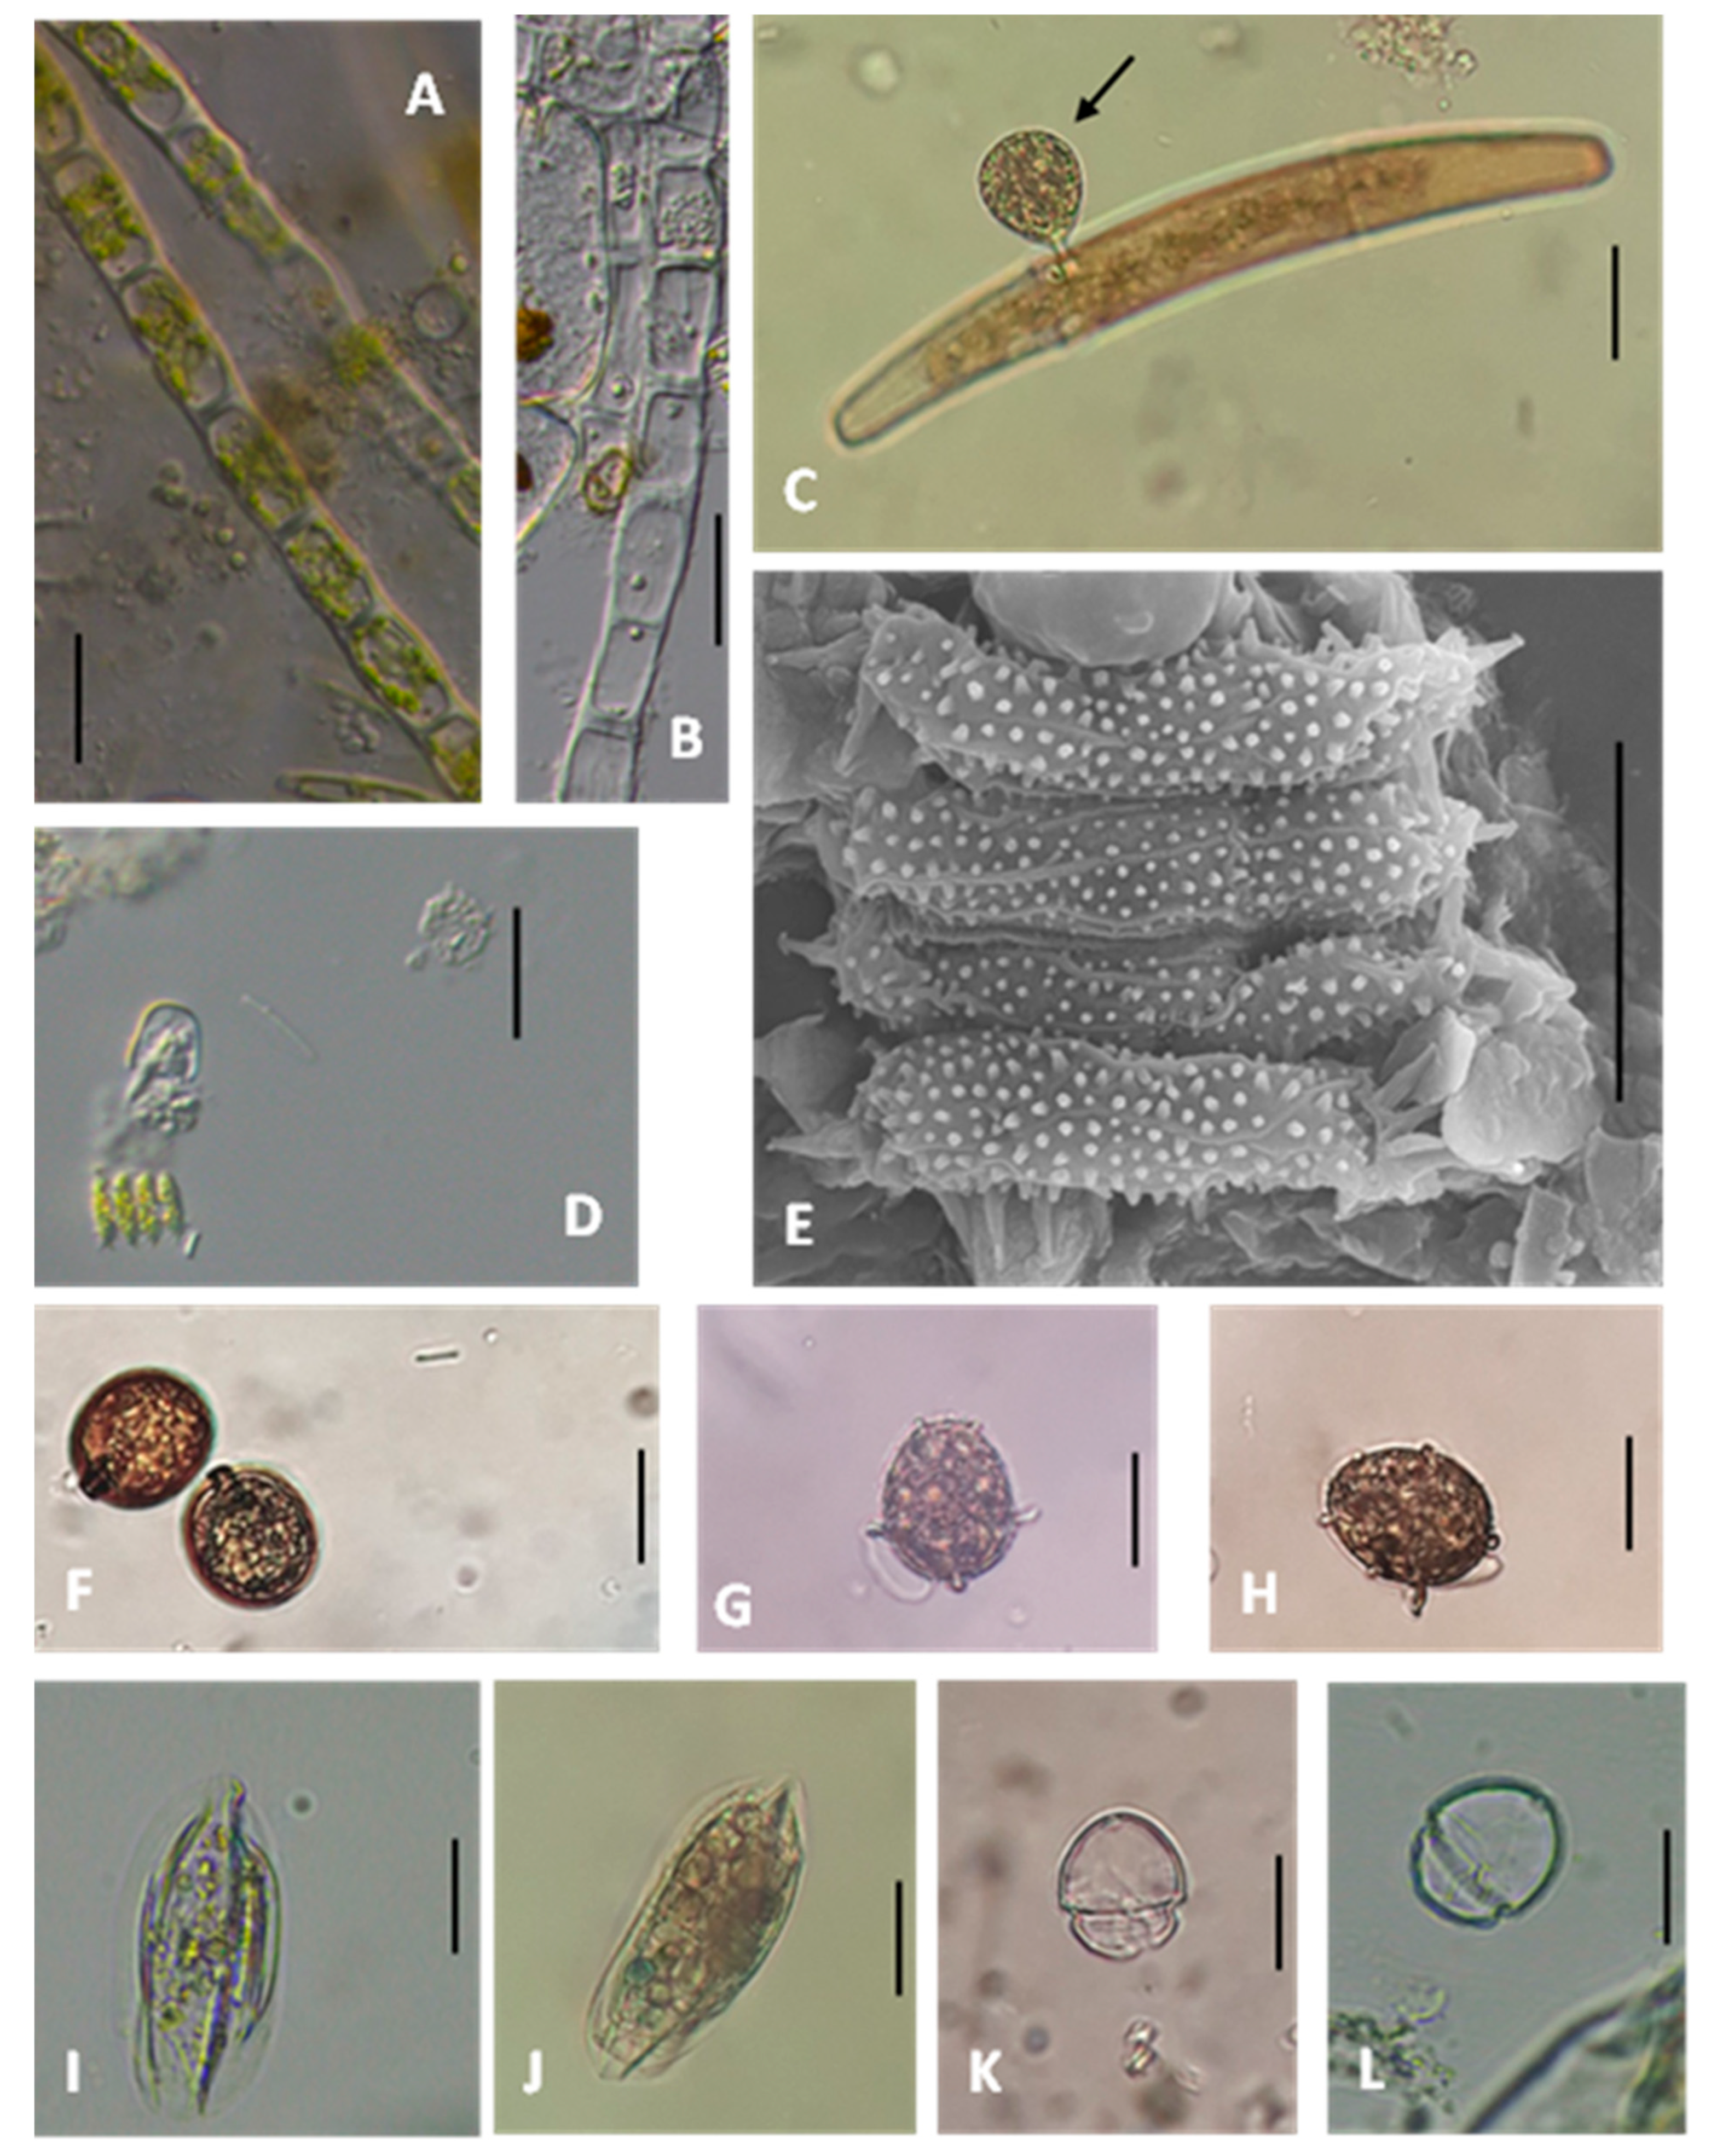
Description: Thallus unbranched and filamentous, with moderately thick cell walls (2 μm). The cell is cylindrical, 17 μm in length and 11 μm in diameter. Chloroplast perforated and plate-like, parietal, covering most of the inner cell wall surface (
Figure 7A,B).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in the Ağaçbaşı, Barma, Sazak, and Kabaca-Petek blanket bogs.
Ecology: They are commonly distributed in
Sphagnum bogs, but also occur in lakes and ponds. They are considered a cosmopolitan taxon [
28,
40].
Genus: Characium A.Braun
- 45.
Characium heteromorphum (Reinsch) Wolle 1887: 178
Reinsch [
17], p. 80, pl. 11, Figure 11.
Description: Cells spherical, with granular cytoplasm. A short, narrowed hyaline pedicel about 4 μm long. Cell diameter approximately 20 μm (
Figure 7C).
Habitat: It was recorded epiphytically on Closterium attached to submerged plants in bog pools, Barma Blanket Bog.
Ecology: It was recorded on
Stigeoclonium [
17].
Genus: Desmodesmus (Chodat) S.S.An, T.Friedl and E.Hegewald
- 46.
Desmodesmus serratus (Corda) S.S.An, Friedl and E.Hegewald 1999: 427
Uherkovich et al. [
36], p. 91, pl. 12, Figures 8–13; John et al. [
40], p. 394, pl. 96, Figure B; Fawley et al. [
46], p. 34, Figures 8–38.
Description: Coenobia usually 4-celled (occasionally 2 or 8). Cells arranged in a straight row. The cell is 8 μm in length and 2 μm in breadth. Outermost cells with spines arranged in a single row, bearing two more distinct subpolar spines at apices. Inner cells with longitudinal, sometimes irregular, rows of spines often fused into granules; rows continuous but restricted to cell margins (
Figure 7D,E).
Habitat: The species was found as epipelic, epiphytic on submerged plants in bog pools, in the Ağaçbaşı Blanket Bog.
Ecology: It is a cosmopolitan species found in the plankton of various water bodies [
40].
Division: Euglenophyta
Genus: Trachelomonas Ehrenberg
- 47.
Trachelomonas mucosa Svirenko 1914: 637, pl. 19: Figure 21
Islam and Muniruzzaman [
30], p. 116, pl. 1, Figures 23–25; Philipose [
31], p. 341, Figure 13a,b.
Description: Lorica elliptical with cylindrical collar structures about 4 μm long. Surface smooth, brown, surrounded by mucus layer approximately 4 μm thick. The cell is 27 μm in length (including the collar) and 24 μm in breadth (
Figure 7F).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, in the Yılanlıtaş Blanket Bog.
Ecology: Although a rare species, it has a cosmopolitan distribution and has only been recorded from aquatic habitats [
63].
- 48.
Trachelomonas raciborskii var.
incerta Dreżepolski 1925: 221, Figure 55 [
24]
Dreżepolski [
24], p. 221, Figure 55; Wołowski [
39], p. 58, pl. 19, Figure 1; Tolivia et al. [
52], p. 25, Figure 2o.
Description: Broad–oval in shape and finely punctate, with two short conical spines located at both poles. Collar structures absent. The lorica is 26 μm in length and 21 μm in breadth (
Figure 7G,H).
Habitat: It was found as epiphytic on submerged plants in bog pools in Ağaçbaşı Blanket Bog.
Ecology: It was reported by Wołowski [
39] from a karstic pond.
Genus: Calycimonas Christen, 1959
Description: According to AlgaeBase, this genus currently includes only one accepted species [
55]. The cells are oval (not flattened), colorless, and phagotrophic flagellates. They possess a rigid body with eight conspicuous spiral ridges. Cells are 25–70 μm long and bear a single flagellum emerging from a subapical canal opening.
Remark: Although it resembles the genus
Tropidoscyphus F. Stein morphologically, it differs by having only one flagellum. Furthermore, the morphologically similar genus
Petalomonas F. Stein can be distinguished from
Calycimonas by being strongly dorsoventrally flattened [
26,
55].
- 49.
Calycimonas physaloides H.R.Christen 1959: 299, Figure 7
Christen [
26], p. 299, Figure 7.
Description: Cells resembling the fruit of
Physalis alkekengi L. [
26], from which the species name derived. Cells nearly ovoid, rigid, bearing eight longitudinal spiral ridges. The posterior end broad and laterally rounded, with distinct terminal point from which longitudinal ridges protrude. Single flagellum slightly shorter than cell body. Cytoplasm containing numerous spherical, green or brownish bodies. The cells are approximately 68 μm in length and 29 μm in breadth (
Figure 7I,J).
Habitat: It was found as epipelic, epiphytic on submerged plants in bog pools, and atmophytic on Sphagnum in the Ağaçbaşı, Yılanlıtaş, Sazak and Kabaca-Petek blanket bogs.
Ecology:
Calycimonas physaloides was first reported from the bottom sediments of eutrophic ponds [
26] and, as in our study, has mostly been recorded in peatland habitats across Europe [
64,
65].
Division: Dinoflagellata
Genus: Opisthoaulax Calado, 2011
Description: The genus
Opisthoaulax is reported for the first time from Türkiye in the present study. According to AlgaeBase, seven taxonomically described and accepted species are currently recognized within the genus [
55]. They are free-living, phagotrophic dinoflagellates lacking chloroplasts. The cells are more or less dorsiventrally flattened, with a length-to-width ratio ranging from 1.1 to 1.6. The epicon is 1.5–2.5 times longer than the hypocone. The cingulum completely encircles the cell [
47,
55].
- 50.
Opisthoaulax vorticella (F.Stein) Calado 2011: 647, Figure 5 [
47]
Christen [
27], p. 335, Figure 21a–h; John et al. [
40], p. 195, pl. 48, fig. B; Calado [
47], p. 647, Figures 5–10.
Description: Cells ovoid and colorless, with conical epicone markedly larger than hypocone; epicone-to-hypocone ratio 3.1. Epicone situated above a broad cingulum. Sulcus (longitudinal groove) slightly extending into epicone and narrowing as it runs toward a point very close to apex of hypocone. The cells are 25 μm in length and 20 μm in breadth; length-to-width ratio 1.3 (
Figure 7K,L).
Habitat: It was reported from epipelic, epiphytic on submerged plants in bog pools, and as atmophytic on Sphagnum in the Ağaçbaşı, Barma, Yılanlıtaş, Sazak, and Kabaca-Petek blanket bogs. It has also been detected in the plankton of Sazak Blanket Bog.
Ecology: This species occurs in peat bogs, ponds, small pools, and meltwater from snow [
40].