Article

Impacts of Fermented Distillers Grains Inclusion on Growth Performance, Nutrient Digestibility, Rumen Fermentation, and Gut Microbiota of Crossbred Simmental Steers


1
Research Center for Bio-Feed and Molecular Nutrition, College of Animal Science and Technology, Southwest University, Chongqing 400715, China
2
Key Laboratory of Animal Nutrition and Bio-Feed, Chongqing Municipal Education Commission, Chongqing 400715, China
3
National Engineering Technique Research Center for Biotechnology, State Key Laboratory of Materials-Oriented Chemical Engineering, College of Biotechnology and Pharmaceutical Engineering, Nanjing Tech University, Nanjing 210009, China
4
College of Agronomy and Biotechnology, Southwest University, Chongqing 400715, China
5
Luzhou Laojiao Co. Ltd., Luzhou 646000, China
*
Author to whom correspondence should be addressed.
†
These authors contributed equally to this work.
Agriculture 2026, 16(19), 2131; https://doi.org/10.3390/agriculture16192131

Submission received: 3 September 2026 / Revised: 26 September 2026 / Accepted: 28 September 2026 / Published: 1 October 2026
(This article belongs to the Special Issue Nutrient Metabolism and Its Role in Livestock Production)

Abstract

This study evaluated the effects of dietary incorporating with fermented distillers grains (FDGs) on growth performance, nutrient digestibility, rumen fermentation, and ruminal/fecal microbiota in crossbred Simmental steers. During a 28-day feeding trial, 36 steers were randomly assigned to control (basal diet only), 4%, and 8% FDG groups, with FDG supplemented on a dry matter basis. Dietary treatments did not alter growth performance or total tract apparent nutrient digestibility. However, 8% FDG improved ruminal neutral detergent fiber (NDF) digestibility and elevated ruminal concentrations of microbial crude protein (MCP), propionic acid, valeric acid, and total volatile fatty acids, shifting fermentation toward a propionate-oriented profile. High-throughput sequencing demonstrated that 8% FDG increased ruminal alpha diversity and altered beta-diversity community structure. Spirochaetota abundance decreased, whereas Cyanobacteriota and Rikenellaceae_RC9_gut_group abundance increased. Redundancy and Spearman correlation analyses identified six upregulated genera, notably Saccharofermentans and an unclassified genus within Victivallaceae, which strongly drove propionate, valerate, and MCP levels. PICRUSt2 predictions revealed enrichment of interconnected pathways involved in nucleotide, carbohydrate, and amino acid metabolism. Fecal microbiota had stable alpha diversity, with only selective enrichment of the phylum Bacillota. In conclusion, 8% FDG restructured ruminal microbial, enhancing fiber degradation and propionate-oriented fermentation efficiency while maintaining hindgut homeostasis.

1. Introduction

The global livestock sector faces a critical dual challenge: meeting the rapidly growing demand for animal proteins (projected to increase 60% for meat and 57% for milk by 2050) while reducing reliance on conventional feed grains that compete directly with human food security [1]. Feed accounts for 60–70% of total operational costs in beef cattle production. Therefore, procuring inexpensive, nutritionally balanced feedstuffs is a primary determinant of economic viability and environmental sustainability in ruminant agriculture. In this context, agro-industrial by-products from microbial bioprocessing have emerged as potential dietary supplements that can convert low-value residues into high-quality animal feed. This process minimizes waste and ensures a closed nutrient loop [2,3].
Distillers grains (DGs) are the primary solid by-product of industrial ethanol and liquor production. Among the most abundant agro-industrial byproducts worldwide, DGs from baijiu (Chinese white liquor) alone exceed 4 million tons annually in China. This massive volume has severe environmental consequences and poses a logistical disposal challenge because of its high moisture content, low pH, and rapid susceptibility to spoilage [4,5]. However, DGs contain high levels of crude protein (CP), residual starch, and minerals; therefore, incorporating them into ruminant diets is potentially one of the most practical and economically viable disposal pathways [6,7]. However, inherent nutritional limitations constrain the applicability of DGs as feed. First, incorporating rice husks as a fermentation matrix in baijiu production generates high crude fiber (CF) and lignocellulose content, restricting voluntary dry matter intake and total-tract nutrient digestibility [8]. Second, excessive acidity (pH < 3.5) from high DG concentrations compromises palatability and potentially perturbs ruminal fermentation homeostasis. Third, DGs contain anti-nutritional factors, including phytic acid, tannins, and residual ethanol. Fourth, mycotoxins—notably aflatoxin B1 and deoxynivalenol—concentrate in DGs and can contaminate feedstock [9,10]. These constraints have limited the permissible inclusion rates of DGs in beef cattle total mixed rations and stimulated considerable interest in developing processing technologies that can improve the feeding value of this abundant agro-industrial byproduct. Microbial fermentation alters DGs’ nutritional composition, reduces anti-nutritional factors and mycotoxins, and accumulates bioactive metabolites. Thus, using fermented distiller’s grains (FDGs) is a promising way to improve the feeding value of raw DGs [11,12].
Emerging evidence has highlighted the physiological and functional benefits of FDG in ruminant nutrition. Replacing 20% of dietary concentrate with probiotic FDGs for 45 days significantly elevated ruminal enzyme activities, raised glycerophospholipid levels, and enriched beneficial taxa (e.g., Prevotella_1 and Bifidobacterium) in finishing cattle [13]. A companion multi-omics investigation further showed that FDGs expanded fecal cellulose-degrading populations and upregulated bile secretion pathways without compromising fecal microbial diversity or stability [14]. Additionally, FDG diets improved systemic immune status while altering the metabolomic profiles of the spleen and mesenteric lymph nodes [15]. This result confirmed that FDGs exert immunomodulatory effects beyond simple nutrient provision.
Despite these advances, few studies have directly evaluated whether FDGs improve key factors related to gut health and growth. Furthermore, the optimal FDG inclusion rate under controlled feeding conditions remains undefined. Consequently, the optimal FDG inclusion rate in the feed for maximizing production efficiency while maintaining ruminal health and physiological homeostasis remains unclear.
Therefore, this study evaluated growth performance, apparent nutrient digestibility, rumen fermentation characteristics, and ruminal and fecal microbiota in crossbred Simmental beef steers fed diets with different FDG inclusion levels. Because established inclusion recommendations were limited, 4% and 8% were chosen as exploratory moderate and relatively high inclusion levels under practical diet formulation constraints, with corresponding adjustments to conventional distiller’s grains, forage hay, and other feed ingredients. We hypothesized that FDG-containing diets would alter rumen fermentation and be associated with shifts in ruminal bacterial community structure. These findings provide an initial empirical basis for future optimization of FDG use in beef cattle production, with potential economic and environmental benefits.

2. Materials and Methods

2.1. Feed Ingredients

This study used FDGs from Nanjing High Tech Institute of Biotechnology (Nanjing, China). Table 1 presents their nutritional composition before and after fermentation.

2.2. Experimental Design

The experiment was conducted on 20 October 2025 in Nanchuan, Chongqing, China. The trial lasted for 35 days, consisting of a 7-day adaptation period and a 28-day formal experimental period. Thirty-six healthy crossbred steers with similar body weights (p > 0.05) were selected and randomly divided into three groups of twelve steers each. The average initial body weights were 343.96 kg for the control group, 336.96 kg for the 4% group, and 334.96 kg for the 8% group, respectively. The cattle were assigned to diets formulated to contain 0% (control), 4% (4% group), or 8% (8%group) FDG on a dry matter basis, with corresponding adjustments to the ingredient composition. Nutritional requirements were based on the NRC (2001) [16] (see Table 2 for dietary ingredients and nutrient composition). Steers were individually housed in a standardized, semi-open barn with tie-stalls containing separate feed bunks and water troughs; this separation ensured independent intake calculations. Total mixed rations were divided into three equal portions and fed to the steers at 07:00, 12:00, and 18:00. Steers were tethered during feeding. Dry matter intake (DMI) per steer was calculated as the difference between feed provided and the amount remaining each day. The barn had natural lighting and ventilation, and feces were removed daily to maintain a hygienic environment.

2.3. Sample Collection and Chemical Analysis

2.3.1. Growth Performance

The fasting body weight of each steer was measured on days 1 and 28 of the formal trial period to calculate average daily gain (ADG). The offered feed and residual feed of each steer were accurately recorded daily, from which the DMI was determined and recorded. The F/G (feed-to-gain ratio) was calculated using the following equation:
F/G = DMI/ADG
where DMI represents dry matter intake (kg/day), and ADG is the average daily gain (kg/day).

2.3.2. Apparent Nutrient Digestibility

Fecal samples (~300 g each) were collected from each steer at 09:00, 13:00, and 19:00 on days 26–28 of the experimental period. Fecal samples from three sampling time points were thoroughly pooled; approximately 100 g was weighed and then combined with a 10% sulfuric acid solution to fix nitrogen. The fecal samples were stored at −20 °C. Fecal samples from each steer were pooled and dried. During the same sampling period, approximately 100 g samples of TMR prior to feeding and residual feed from each steer were collected. After collection, the pre-feeding feed and residual feed from each steer were combined to form composite samples. The fecal and feed samples were dried at 65 °C and ground for subsequent analysis. Dry matter, CP, neutral detergent fiber (NDF), acid detergent fiber (ADF), phosphorus, and calcium contents were determined separately in fecal and feed samples. Hydrochloric acid-insoluble ash (AIA) content was used as an indicator of each nutrient’s apparent digestibility, calculated as follows:
Apparent digestibility (%) = 100 − (AIA content in diet/AIA content in feces) × (nutrient content in feces/nutrient content in diet) × 100

2.3.3. Rumen Fermentation Parameters

On day 28 of the formal experimental period, six steers were randomly selected from the twelve experimental animals in each group before morning feeding. These selected steers were a subset of the twelve animals used for growth-performance recording and fecal sampling, and no additional animals were used. Following restraint under fasting conditions, ruminal fluid was collected via an oesophageal-tube rumen fluid sampler. Approximately the first 200 mL of ruminal fluid was discarded to avoid salivary contamination. The remaining fluid was filtered through four layers of gauze, aliquoted, and transported to the laboratory at low temperature for storage at −80 °C.
Rumen fluid pH was measured using a portable pH meter (Testo 206-pH, Shenzhen Testo Instrument; Shenzhen, China). NH3-N content was determined by the indophenol colorimetric method, and microbial protein (MCP) content was determined using Coomassie brilliant blue. Briefly, 1 mL of ruminal fluid was centrifuged at 12,000× g for 10 min at 4 °C. For NH3-N determination, 40 μL of the supernatant was transferred into a 10 mL centrifuge tube, mixed with 2.5 mL phenol solution and 2 mL sodium hypochlorite solution, vortexed, and incubated in a water bath at 37 °C for 30 min. Afterward, transfer 200 μL of the reaction mixture into a microplate, and read the absorbance at 630 nm using a microplate reader (Synergy H1, BioTek Instruments, Winooski, VT, USA). The NH3-N concentration was calculated against the standard curve. For MCP measurement, 5 μL of supernatant was added to a microplate well with 250 μL Coomassie Brilliant Blue solution. Absorbance was measured at 595 nm, and MCP content was calculated using the standard curve [18,19,20]. Volatile fatty acid (VFA) content was determined using an internal standard method. In brief, 1 mL ruminal fluid was pipetted into a 1.5 mL centrifuge tube, mixed with 200 μL metaphosphoric acid deproteinizing solution, and vortexed. The mixture was centrifuged at 12,000× g for 10 min at 4 °C. The supernatant was drawn with a 1 mL syringe, filtered through a 0.22 μm filter membrane into a sample vial, and analysed using a gas chromatograph (Shimadzu 2010 Plus, Shimadzu Corporation, Kyoto, Japan). Peak areas were used for quantification with crotonic acid as the internal standard [21,22].

2.3.4. Microbial Diversity

Rumen fluid and fecal samples stored at –80 °C were shipped on dry ice to Majorbio Bio-Pharm Technology (Shanghai, China) for high-throughput 16S rRNA gene sequencing (primers 338F_806R). Raw sequencing data were quality-filtered, denoised, and processed to generate amplicon sequence variants (ASVs). Based on the normalized ASV feature table, downstream bioinformatic and statistical analyses were performed, including α- and β-diversity, taxonomic composition, differentially abundant taxa, and functional predictions.

2.3.5. Determination of Nutritional Composition

CP content was determined using a fully automatic Kjeldahl nitrogen analyzer (Model K1160, Shandong Haineng Scientific Instrument; Jinan, China) in accordance with GB/T 6432—2018 [23]. Additionally, NDF and ADF contents were determined using a fully automatic fiber analyzer (Model F2000, Shandong Haineng Scientific Instrument; Jinan, China) in accordance with GB/T 20806—2022 [24] and NY/T 1459—2022 [25], respectively. Methods from GB/T 6436—2018 [26] and GB/T 6437—2018 [27] were used to measure Ca and P content, respectively. Finally, crude ash content was measured in a muffle furnace (Model SX-G18122, Tianjin Zhonghuan Electric Furnace; Tianjin, China), following GB/T 6438—2007 [28].

2.4. Data Statistics and Analysis

Data were processed in Microsoft Excel 2019. Statistical analyses of growth performance, apparent digestibility, and rumen fermentation parameters were performed in R (v4.3.3). Normality of model residuals and homogeneity of variance were evaluated using the Shapiro–Wilk test (shapiro.test function) and Levene tests (in the car package), respectively. A one-way analysis of variance (ANOVA) was conducted using the aov function, followed by Tukey’s honestly significant difference (HSD) test for multiple comparisons. Orthogonal polynomial contrasts were incorporated into the ANOVA to evaluate linear and quadratic responses across the equally spaced FDG inclusion levels (0%, 4%, and 8% of dietary DM). Contrast coefficients were proportional to −1, 0, and 1 for the linear effect and 1, −2, and 1 for the quadratic effect. A significant linear effect indicated a progressive response with increasing FDG inclusion, whereas a significant quadratic effect indicated a nonlinear response in which the 4% group deviated from the linear trend between the 0% and 8% groups. For data that violated the assumption of normality or homogeneity of variance, including the relative abundance of rumen fluid and feal microbiota, the Kruskal–Wallis test (kruskal.test function) was used, followed by Dunn’s multiple comparison test (Dunn test function from the FSA package). The Bonferroni correction was applied for p-values. Data were expressed as the mean and standard error of the mean (SEM). Significance was set at p < 0.05.
Microbial community-environment associations were analyzed using the vegan R package. α-diversity indices were calculated from the ASV abundance matrix and compared among the three groups using the Kruskal–Wallis test, followed by pairwise Wilcoxon rank-sum tests with Benjamini–Hochberg correction. Principal coordinate analysis (PCoA) based on Bray–Curtis distances was used to assess variation in community structure. Overall and pairwise differences were tested using PERMANOVA (adonis2, 9999 permutations), with R2 values reported and pairwise p values adjusted using the Benjamini–Hochberg procedure. Homogeneity of multivariate dispersion was assessed using PERMDISP with 9999 permutations. Relative abundances of the top 10 dominant phyla and genera were obtained. Differentially abundant genera were screened using the DESeq2 package (Padj < 0.05, |log2 fold-change| > 1). Core mechanistic bacterial genera were identified as those that were correlated (p < 0.05, Spearman’s rho, Hmisc package) with altered fermentation parameters (Wilcoxon test, p < 0.05); the results were visualized using the pheatmap package. In vegan, a redundancy analysis (RDA) model was constructed using the Hellinger-transformed genus matrix against altered fermentation indicators. Overall model significance was evaluated using 999 Monte Carlo permutation tests.
Functional prediction and association network analyses were performed in Python (v3.12.13). PICRUSt2 was used to predict KEGG Orthology (KO) abundance. Differences in functional contribution at the genus level (Δ = KOtreatment − KOcontrol) was calculated to plot a genus–KO clustering heatmap. Next, mapping differential genera to KEGG pathways generated an association network diagram, with node size representing the magnitude of functional contribution and edge width representing the association strength.

3. Results

3.1. Effect of FDGs on Growth Performance

None of the growth performance indicators differed significantly among the groups (p > 0.05; Table 3).

3.2. Effect of FDGs on Apparent Digestibility

The 8% group had significantly higher NDF digestibility than the control group (p < 0.05), but the 4% group did not (p > 0.05) (Table 4). In addition, NDF digestibility had a quadratic relationship with increasing FDGs (pQuadratic < 0.05). Between-group differences were absent in the apparent digestibility of DM, CP, ADF, P, and Ca (p > 0.05).

3.3. Effect of FDGs onRumen Fermentation Parameters

The 8% group had higher MCP, propionic acid, and valeric acid contents than the control group (p < 0.05; Table 5). The 4% group had higher valeric acid content but lower acetic acid content and a lower acetic acid-to-propionic acid ratio than the control (p < 0.05). Acetic acid and total VFA contents were also higher in the 8% group than in the 4% group (p < 0.05). As FDGs increased, acetic and valeric acid contents and the ratio of acetic to propionic acid contents increased linearly (PLinear < 0.05), whereas propionic acid content had a quadratic response (PQuadratic < 0.05), MCP content showed linear and quadratic response trends (PLinear = 0.051, PQuadratic = 0.054), and valeric acid content showed quadratic response trends (PQuadratic = 0.065).

3.4. Effect of FDGs on Rumen Microbial Community Structure

3.4.1. Rumen Fluid α-Diversity

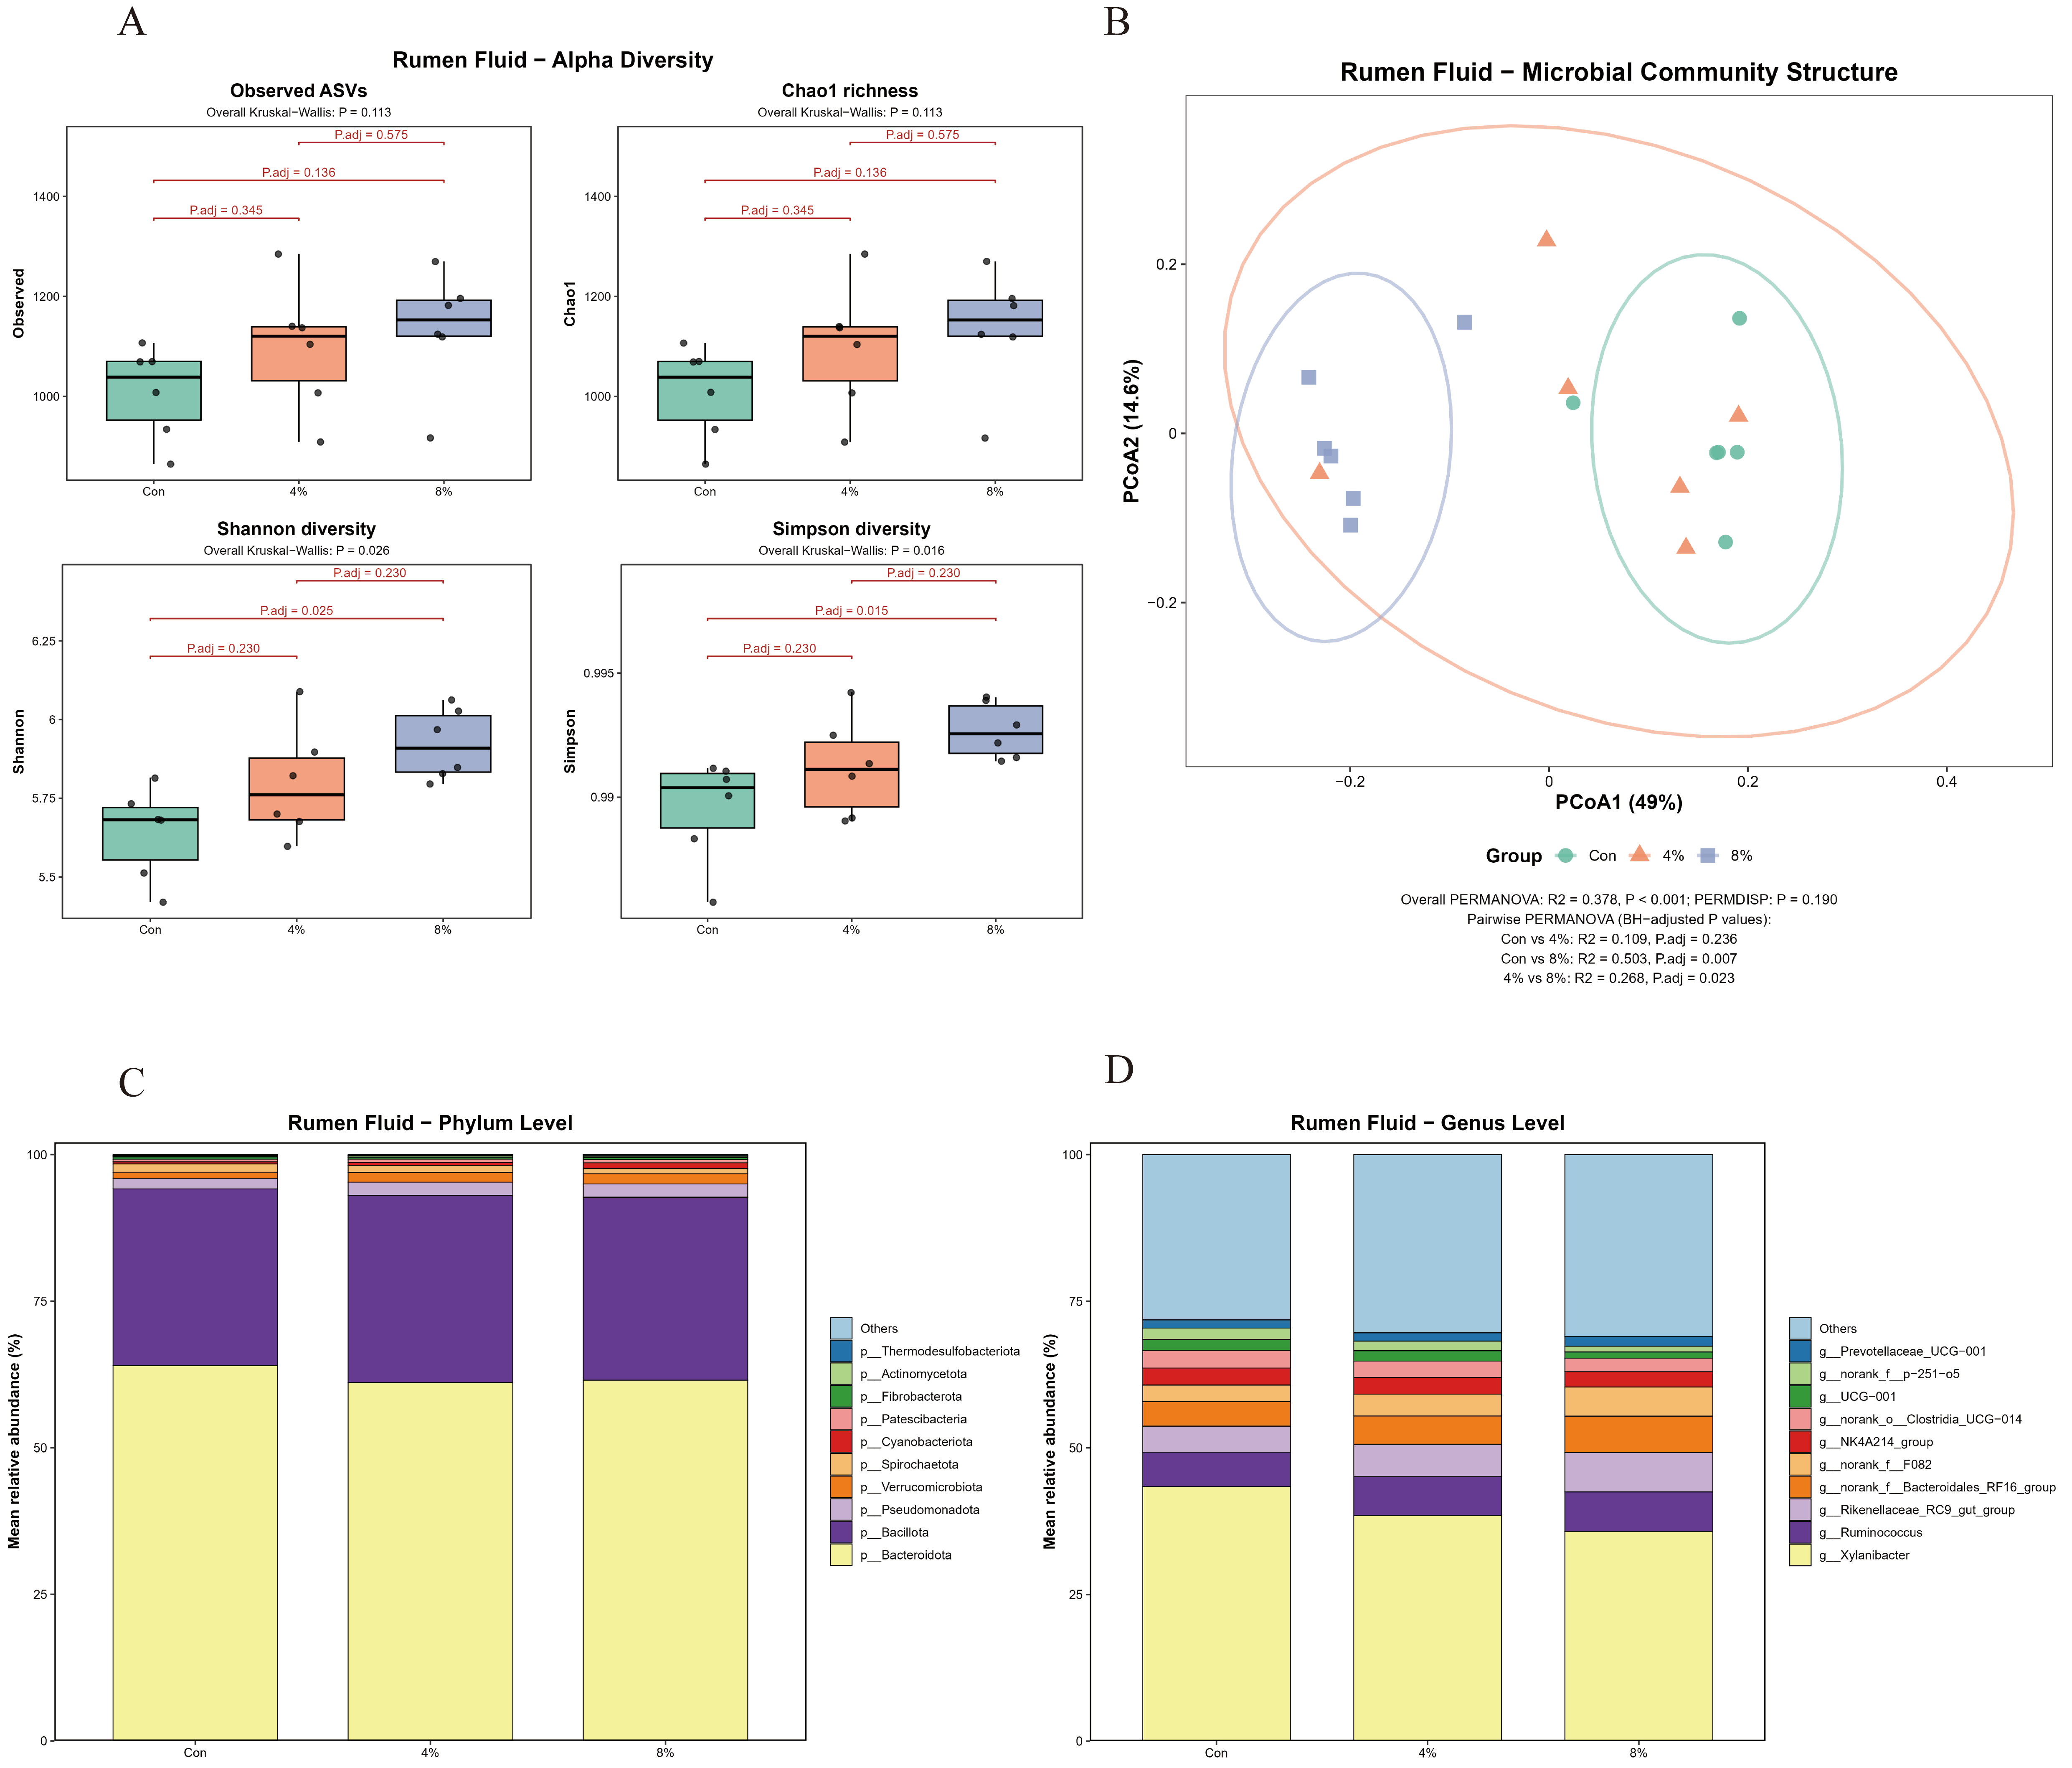
The observed ASV and Chao1 richness indices did not differ significantly among the three treatment groups (p > 0.05). In contrast, the Shannon (p < 0.05) and Simpson (p < 0.05) diversity indices differed significantly overall. The Shannon, and Simpson indices were higher in the 8% group than in the control (adjusted p < 0.05), but they did not differ between the 4% and control groups (adjusted p > 0.05). These indices also did not differ between the 4% and 8% groups (adjusted p > 0.05) (Figure 1A).

3.4.2. Rumen Fluid β-Diversity

The PCoA results showed distinct clustering of rumen microbial communities in the control, 4%, and 8% groups (Figure 1B). The overall microbial community composition differed significantly among the three groups (PERMANOVA, R2 = 0.378, p < 0.001). Pairwise PERMANOVA with Benjamini–Hochberg correction showed significant differences between the control and 8% groups (R2 = 0.503, adjusted p = 0.007) and between the 4% and 8% groups (R2 = 0.268, adjusted p = 0.023). In contrast, no significant difference was detected between the control and 4% groups (R2 = 0.109, adjusted p = 0.236). Multivariate dispersion did not differ significantly among the three groups (PERMDISP, p = 0.190), these results indicate that differences in rumen microbial community composition were most pronounced in cattle fed the diet containing 8% FDG.

3.4.3. Microbial Abundance Analysis

Analysis of the top 10 most abundant phyla in rumen fluid revealed that Spirochaetota abundance decreased from control levels in the 8% group (p < 0.05), while Cyanobacteriota abundance increased (p < 0.05). However, the 4% group showed no significant differences from control (p > 0.05) (Table 6; Figure 1C,D).
Among the top 10 genera in rumen fluid, Rikenellaceae RC9 gut group abundance was significantly higher in the 8% group than in control (p < 0.05), whereas Clostridia UCG-014 abundance was significantly lower (p < 0.05). Again, the 4% group did not differ from control (p > 0.05). Furthermore, the Rikenellaceae RC9 gut group was significantly more abundant in the 8% group than in the 4% group (p < 0.05).
Figure 1. The effect of different proportions of fermented distiller’s grains on the rumen microbial community structure of cross-bred steers. (A) Alpha diversity indices (Observed ASVs, Chao1, Shannon, and Simpson) of rumen fluid microbiota among the Con, 4%, and 8% groups. Boxes represent the interquartile range, and horizontal lines within boxes indicate medians. Statistical significance was evaluated using the Wilcoxon rank-sum test. (B) PCoA plot based on Bray–Curtis dissimilarities illustrating beta diversity and rumen microbial community structure among treatment groups (PCoA1 = 49.0%, PCoA2 = 14.6%). Each symbol represents an individual sample, and ellipses represent 95% confidence intervals. Overall community composition differed significantly among groups (PERMANOVA, R2 = 0.378, p < 0.001). Pairwise PERMANOVA with Benjamini–Hochberg correction showed significant differences between the control and 8% groups (R2 = 0.503, adjusted p = 0.007) and between the 4% and 8% groups (R2 = 0.268, adjusted p = 0.023), whereas the control and 4% groups did not differ significantly (R2 = 0.109, adjusted p = 0.236). Multivariate dispersion did not differ among groups (PERMDISP, p = 0.190). (C) Stacked bar plot displaying the relative abundance of dominant rumen microbial phyla across treatment groups. (D) Stacked bar plot displaying the relative abundance of the top 10 dominant rumen bacterial genera across treatment groups. Con: Control, diet formulated without fermented distillers’ grains; 4%: 4% group, diet formulated to contain 4% fermented distillers’ grains; 8%: 8% group, diet formulated to contain 8% fermented distillers’ grains (n = 6). Abbreviations: PCoA, principal coordinate analysis.
Agriculture 16 02131 g001

3.4.4. Core Rumen Taxa That Drove Fermentation and Functional Networks

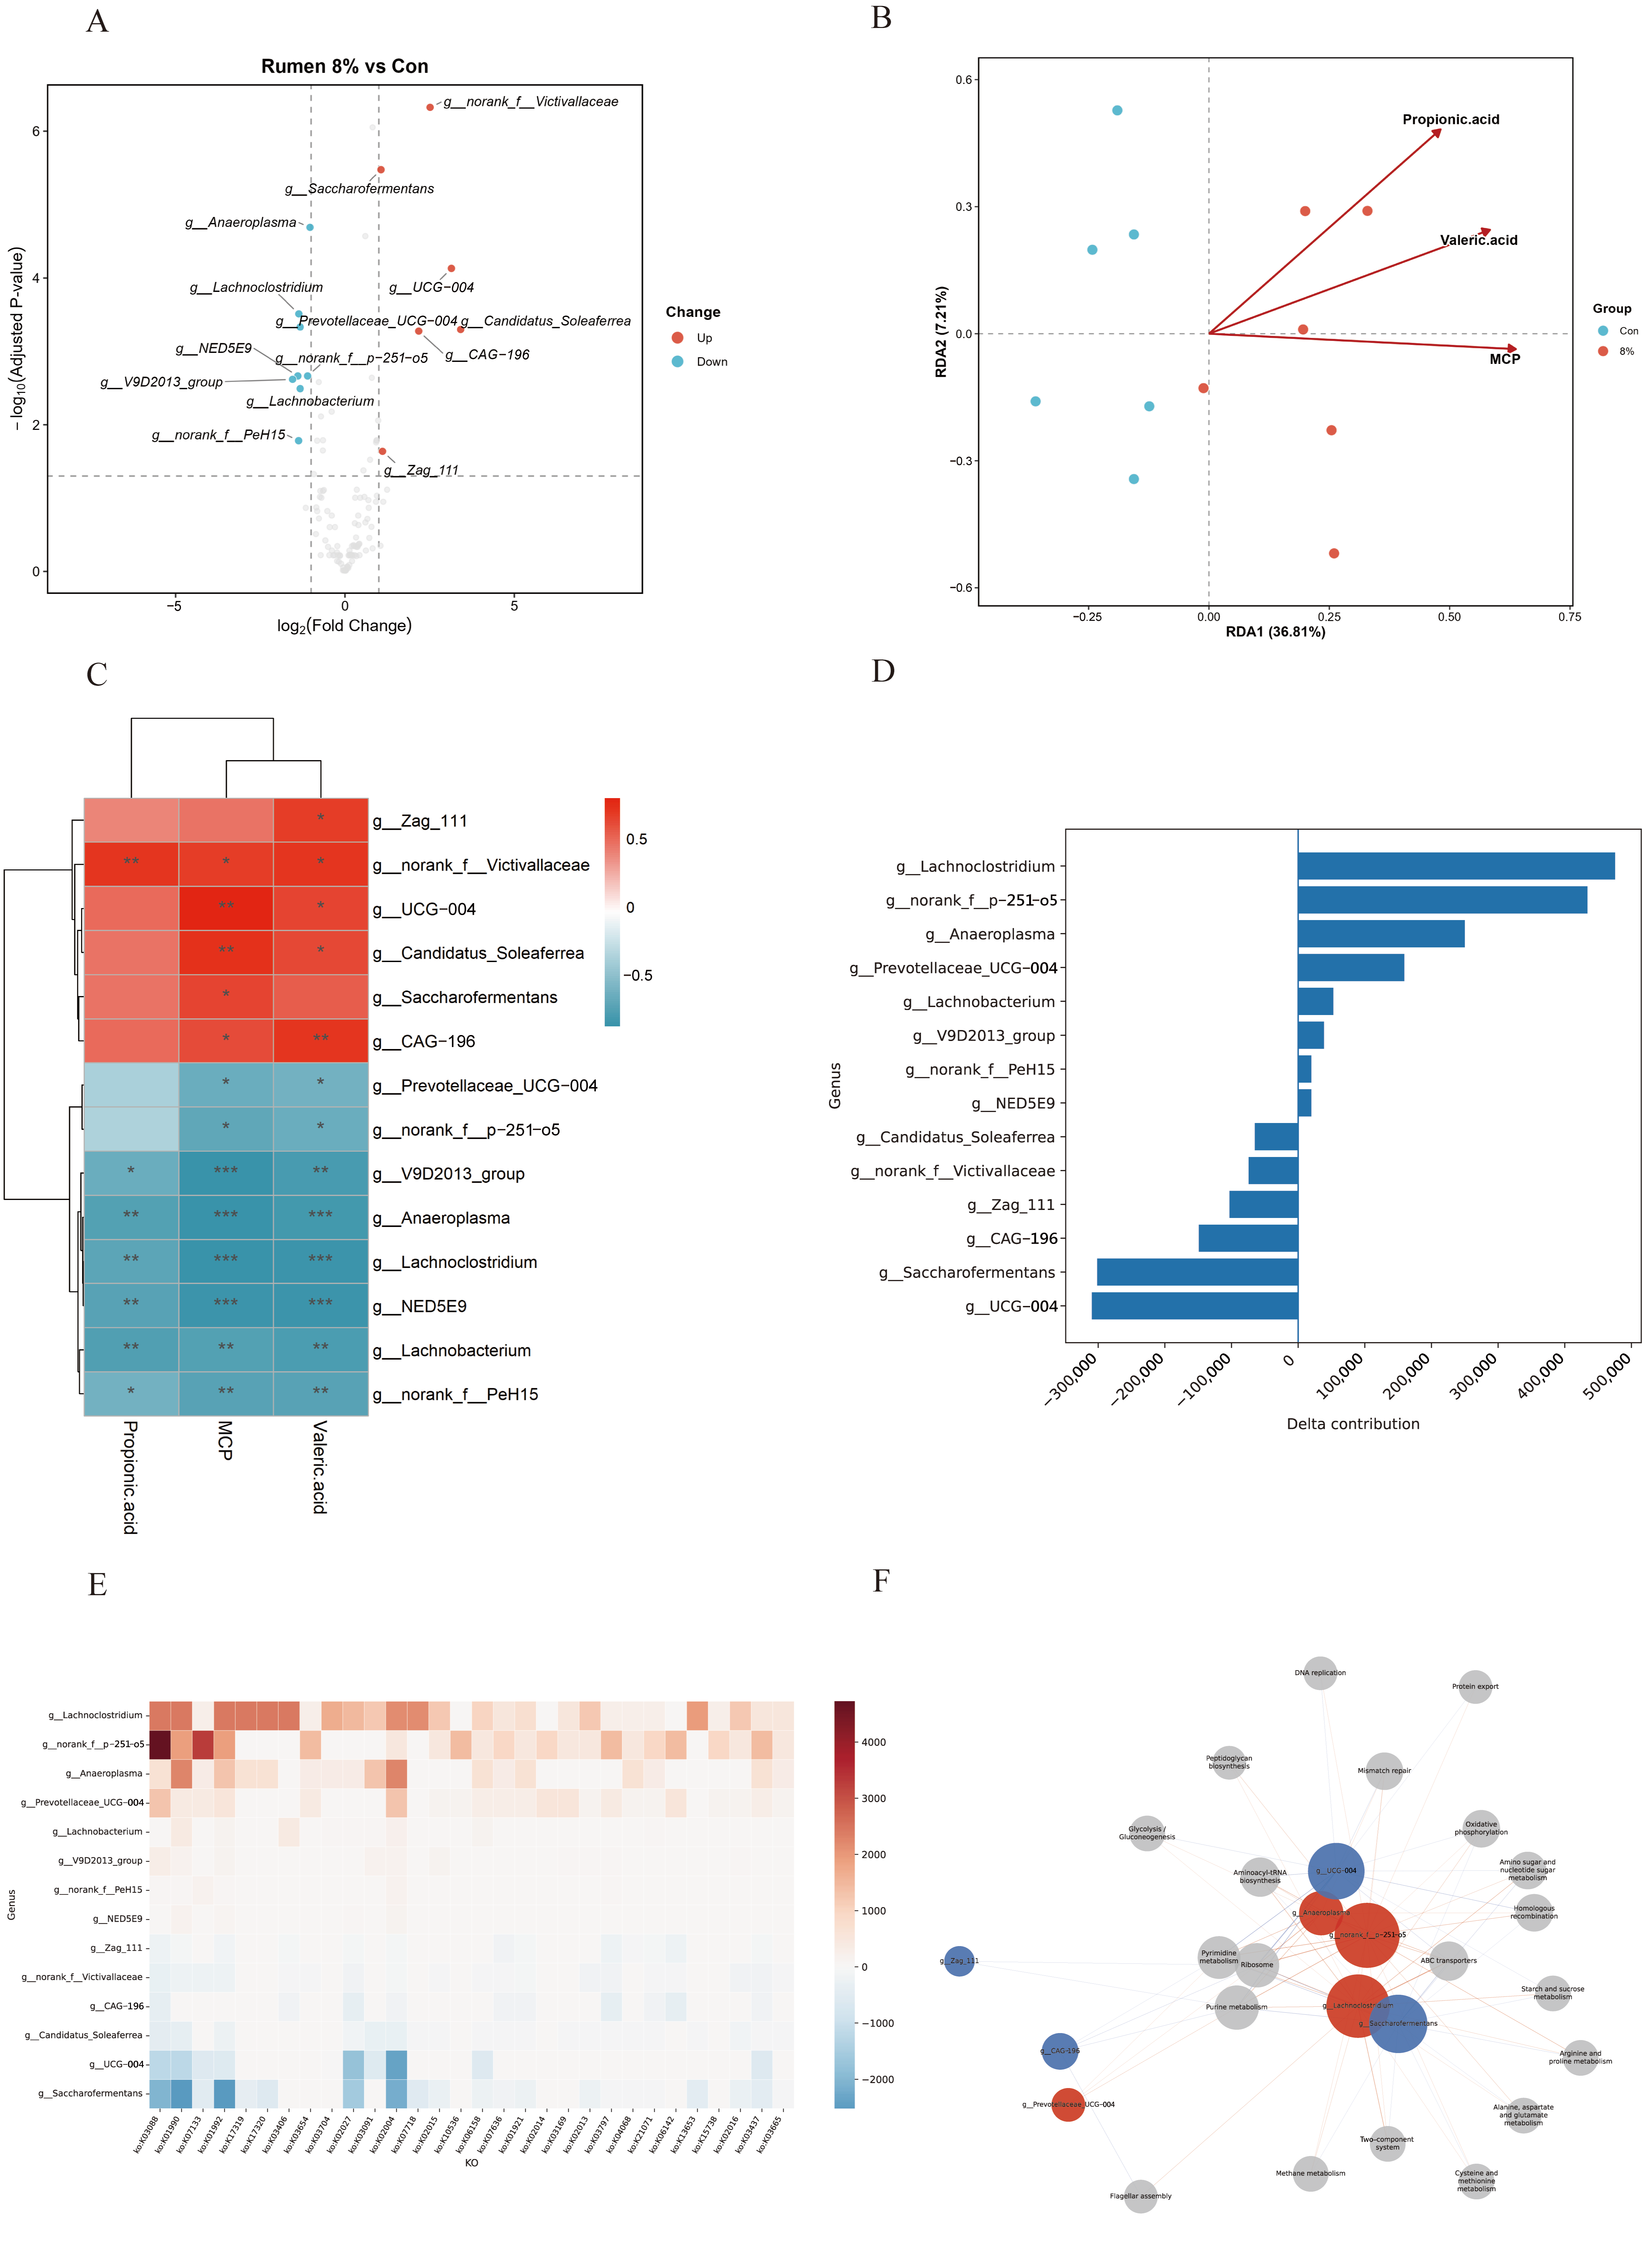
To elucidate the microbiological and functional mechanisms underlying altered fermentation profiles, we evaluated differentially abundant genera and microbial-environmental associations, and predicted functional networks between the control and 8% groups (Figure 2A–F). Differential abundance analysis using DESeq2 identified distinct taxonomic shifts (Padj < 0.05, |log2 fold change| > 1; Figure 2A). The following genera were significantly upregulated in the 8% group: g__norank_f__Victivallaceae, g__Saccharofermentans, g__UCG-004, g__Candidatus_Soleaferrea, g__CAG-196, and g__Zag_111. Conversely, the following genera were significantly downregulated: g__Lachnoclostridium, g__Anaeroplasma, g__Prevotellaceae_UCG-004, g__norank_f__p-251-o5, g__NED5E9, g__V9D2013_group, g__Lachnobacterium, and g__norank_f__PeH15.
The RDA yielded a significant model (F = 2.321, p = 0.024, Monte Carlo permutation test; Appendix A), indicating that selected fermentation parameters (MCP, propionic acid, and valeric acid contents) accounted for 46.54% of the total variance in genus composition. The first two axes explained 36.81% and 7.21% of the total variance, respectively (Figure 2B).
To identify the core bacterial taxa that drove metabolic shifts, we performed Spearman rank correlation analysis on all detected bacterial genera and significantly altered fermentation parameters (MCP, propionic acid, and valeric acid contents; Appendix B). Next, we applied DESeq2 to identify the intersection between significantly correlated genera (p < 0.05) and differentially abundant genera (Figure 2A), yielding the core functional taxa.
Spearman’s rank correlation analysis revealed clear functional partitioning between core bacterial genera and fermentation parameters (Figure 2C). Genera enriched in the 8% group (g__Zag_111, g__norank_f__Victivallaceae, g__UCG-004, g__Candidatus_Soleaferrea, g__Saccharofermentans, and g__CAG-196) were positively correlated with propionic acid, MCP, and valeric acid contents (p < 0.05). In contrast, downregulated genera (g__Prevotellaceae_UCG-004, g__Anaeroplasma, and g__Lachnoclostridium) were negatively correlated with these fermentation parameters (p < 0.05).
We applied PICRUSt2-based functional contribution analysis to quantify genus-specific differences in KO abundance (Figure 2D,E). Notable positive contributors to KOs were g__Lachnoclostridium, g__norank_f__p-251-o5, and g__Anaeroplasma, whereas negative contributors were g__UCG-004, g__Saccharofermentans, and g__CAG-196 (Figure 2D). The genus–KO heatmap further illustrated the predicted relative contributions of differentially abundant genera to specific KO functions (Figure 2E; for detailed functional descriptions of KOs, see Appendix C).
Finally, the bipartite genus–KEGG pathway association network demonstrated that these core genera were associated with important metabolic pathways (Figure 2F). Specifically, nucleotide (pyrimidine and purine) metabolism, carbohydrate (starch and sucrose, amino sugar and nucleotide sugar) metabolism, amino acid (alanine, aspartate, and glutamate; cysteine and methionine) metabolism, and cell structure synthesis (peptidoglycan biosynthesis and ribosomes) were implicated. Collectively, these associations explained the increased propionic acid yield and microbial protein synthesis in the 8% group.

3.5. Effect of FDGs on Fecal Microbial Community Structure

3.5.1. Fecal α-Diversity

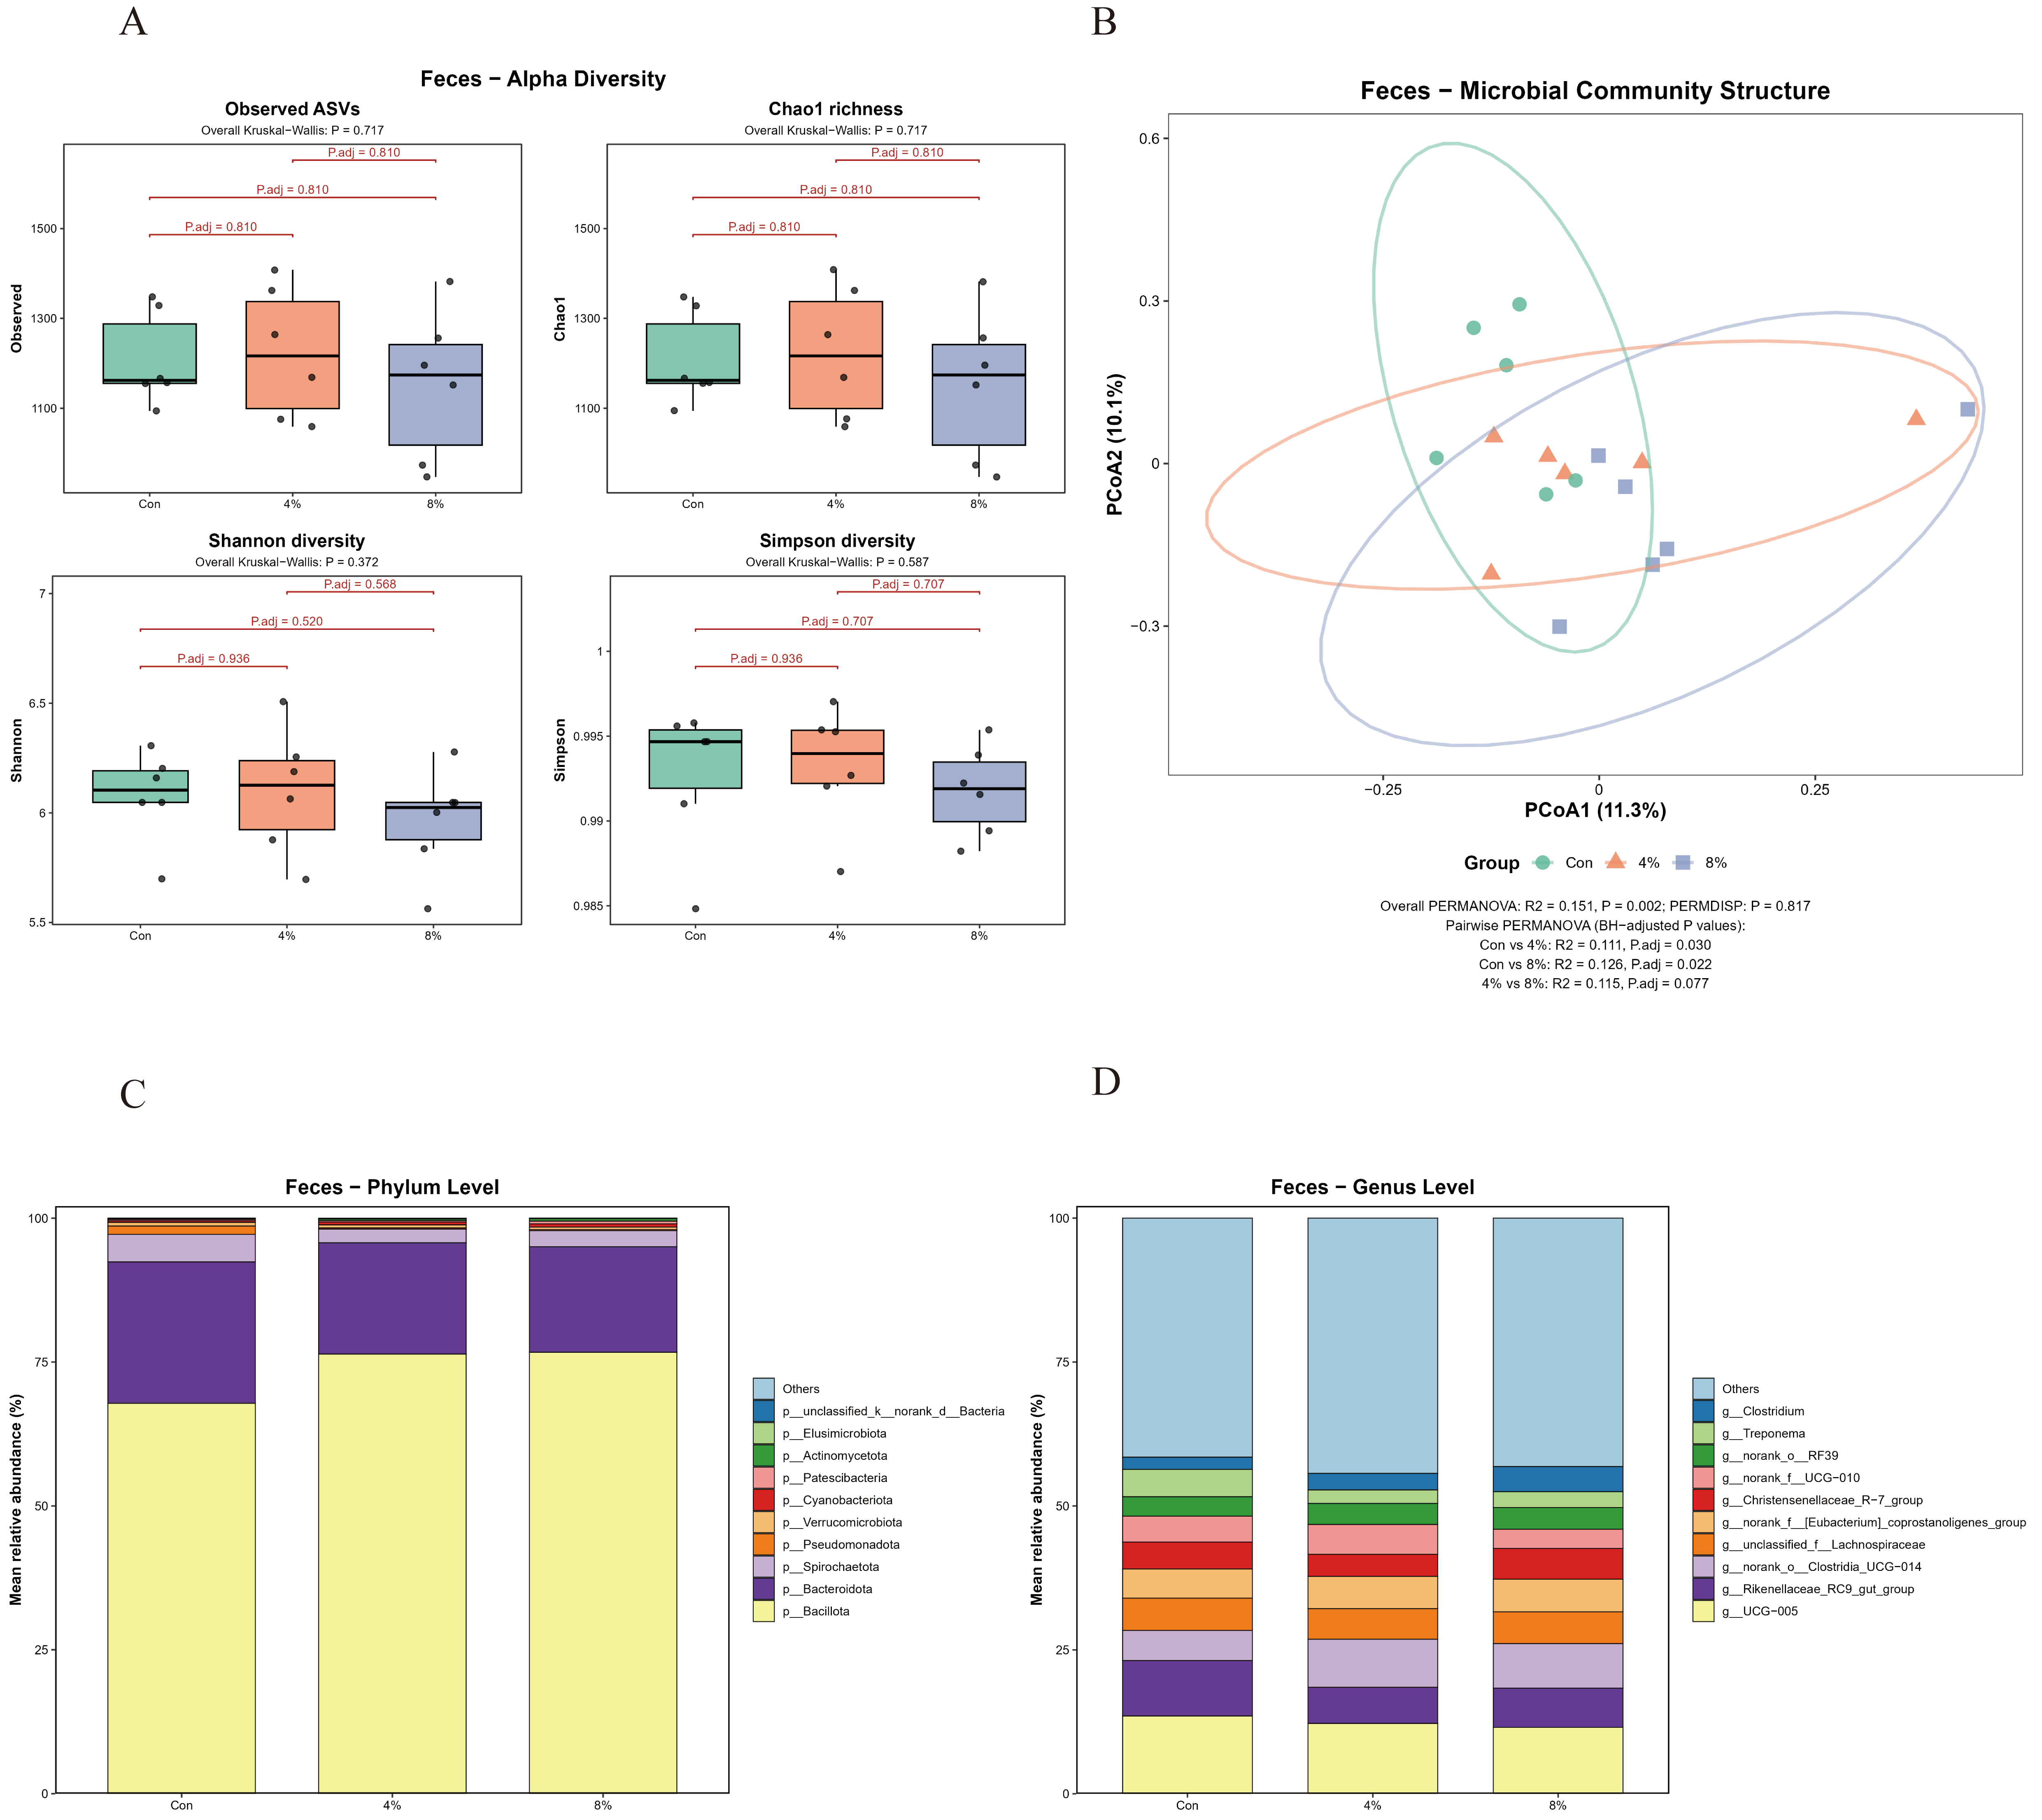
The three groups did not differ in observed ASVs, Chao-1, Shannon, or Simpson indices (p > 0.05; Figure 3A).

3.5.2. Fecal β-Diversity

Rumen microbial communities formed distinct clusters in the control, 4%, and 8% groups (PCoA; Figure 3B). Overall, fecal microbial community composition differed significantly among treatments (PERMANOVA, R2 = 0.151, p = 0.002). Pairwise PERMANOVA with Benjamini–Hochberg correction revealed significant differences between the control and 4% groups (R2 = 0.111, adjusted p = 0.030) and between the control and 8% groups (R2 = 0.126, adjusted p = 0.022). No significant difference was detected between the 4% and 8% groups (R2 = 0.115, adjusted p = 0.077). Multivariate dispersion did not differ significantly among groups (PERMDISP, p = 0.817), indicating that unequal within-group dispersion was unlikely to drive the PERMANOVA results.
Figure 2. Differential microbial taxa and their predicted functional contributions in response to 8% group treatment. (A) Volcano plot illustrating differentially abundant bacterial genera between the Con and 8% groups evaluated by DESeq2 analysis (Padj < 0.05 |log2 Fold Change| > 1). Red and blue dots represent significantly up-regulated and down-regulated genera in the 8% group, respectively. (B) RDA showing the relationship between core bacterial genus composition and significantly altered rumen fermentation parameters (propionic acid, valeric acid, and MCP). Blue and red dots indicate individual samples from the Con and 8% groups, respectively. (C) Spearman rank correlation heatmap between core bacterial genera and rumen fermentation parameters. The color gradient indicates the Spearman correlation coefficient, ranging from blue (negative correlation) to red (positive correlation). Asterisks denote statistical significance. (D) Genus-level differences in predicted KO contributions (Δ = KOtreatment − KOcontrol) inferred using PICRUSt2, showing the direction and magnitude of functional changes associated with individual genera. (E) Heatmap displaying the abundance allocation of core bacterial genera across 30 key KO function nodes (detailed functional descriptions are listed in Table A2). (F) Genus–KEGG pathway association network illustrating the functional links between core bacterial taxa and enriched metabolic pathways. Node sizes represent functional contribution magnitude, and edge widths indicate association strength. Con: control, diet formulated without fermented distillers’ grains; 4%: 4% group, diet formulated to contain 4% fermented distillers’ grains; 8%: 8% group, diet formulated to contain 8% fermented distillers’ grains (n = 6). Asterisks denote statistical significance (* p < 0.05, ** p < 0.01, *** p < 0.001). Abbreviations: RDA, redundancy analysis; MCP, microbial crude protein; KO, KEGG Orthology.
Agriculture 16 02131 g002
Figure 3. Effect of different proportions of fermented distiller’s grains on the microbial community structure of cattle manure. (A) Alpha diversity indices (Observed ASVs, Chao1, Shannon, and Simpson) of fecal microbiota among the Con, 4%, and 8% groups. Boxes represent the interquartile range, and horizontal lines within boxes indicate medians. Statistical significance was evaluated using the Wilcoxon rank-sum test. (B) PCoA plot based on Bray–Curtis dissimilarities illustrating beta diversity and fecal microbial community structure among treatment groups (PCoA1 = 11.3%, PCoA2 = 10.1%). Each symbol represents an individual sample, and ellipses represent 95% confidence intervals. Overall community composition differed significantly among groups (PERMANOVA, R2 = 0.151, p = 0.002). Pairwise PERMANOVA with Benjamini–Hochberg correction showed significant differences between the control and 4% groups (R2 = 0.111, adjusted p = 0.030) and between the control and 8% groups (R2 = 0.126, adjusted p = 0.022), whereas the 4% and 8% groups did not differ significantly (R2 = 0.115, adjusted p = 0.077). Multivariate dispersion did not differ among groups (PERMDISP, p = 0.817). (C) Stacked bar plot displaying the relative abundance of dominant fecal microbial phyla across treatment groups. (D) Stacked bar plot displaying the relative abundance of the top 10 dominant fecal bacterial genera across treatment groups. Con: control, diet formulated without fermented distillers’ grains; 4%: 4% group, diet formulated to contain 4% fermented distillers’ grains; 8%: 8% group, diet formulated to contain 8% fermented distillers’ grains (n = 6). Abbreviations: PCoA, principal coordinate analysis.
Agriculture 16 02131 g003

3.5.3. Species Abundance Analysis

Analysis of the top 10 most abundant phyla in fecal samples revealed that Bacillota abundance was significantly higher in both the 4% and 8% groups than in the control (p < 0.05); however, the abundance did not differ between the 4% and 8% FDG groups (p > 0.05) (Table 7; Figure 3C,D). No significant differences in genus-level abundance were observed among the groups (p > 0.05).

4. Discussion

4.1. Growth Performance and Apparent Nutrient Digestibility

Dietary inclusion of 8% FDGs significantly improved ruminal neutral detergent fiber digestibility without altering overall growth performance or total tract nutrient digestibility in crossbred cattle. The lack of change in growth performance, despite improvements in average daily gain and feed conversion efficiency, may largely reflect the relatively short 28-day feeding period. This duration may be insufficient for translating ruminal metabolic optimization into measurable weight gain. Previous research supports this hypothesis, showing that ruminal microbial and host physiological adaptations to dietary transitions in cattle require more than 4 weeks to fully stabilize [29]. Similarly, a study investigating FDG inclusion for 45 days found that the treatment enhanced rumen fermentation parameters and enzymatic activities without altering growth performance [13]. These results imply that the primary benefit of fermented feeds lies in optimizing ruminal health rather than driving rapid muscle deposition.
Two complementary mechanisms can explain the selective enhancement of fiber degradation capacity. First, solid-state probiotic pre-digestion produces FDGs with lower baseline fiber content because recalcitrant structural carbohydrates are degraded into easily fermentable substrates [30]. Second, dietary supplementation reshapes the rumen microbial ecosystem toward a fibrolytic bacteria-enriched state, expanding the host’s endogenous fiber-degrading capacity. This bifactorial framework aligns with the model proposed by Firkins and colleagues [31]. They emphasized that dietary enhancement of fiber digestibility results from a synergy between pre-cleavage substrates and enriched fibrolytic consortia expressing carbohydrate-active enzymes. Similarly, microbial pretreatment of fibrous residues using Saccharomyces cerevisiae, Aspergillus niger, and fibrolytic enzymes significantly reduced structural fibers and increased ruminal degradability [32].

4.2. Rumen Fermentation Parameters

The rumen microbiota is the central metabolic engine, converting indigestible plant cell walls into VFAs. This process supplies up to 70% of the host’s maintenance energy and synthesizes microbial proteins—the chief source of absorbable amino acids in ruminants [33,34]. Here, we observed that FDG inclusion, particularly at 8%, significantly increased ruminal concentrations of MCP, propionic acid, valeric acid, and total volatile fatty acid contents, shifting fermentation toward a propionate-oriented pattern. The enhanced propionate yield is physiologically important, as propionate is the primary gluconeogenic precursor in ruminants and supplies 60–70% of hepatic glucose synthesis [35]. A mechanistically parallel response has been reported [36], where dietary supplementation significantly increased ruminal propionate concentration and microbial protein yield in vitro. This change was accompanied by enrichment of Prevotella and Prevotellaceae_UCG-004, both closely associated with propionogenesis and protein assimilation. In our study, the simultaneous increase in MCP and propionate supports the reported model, showing that FDGs promote energy-efficient propionate production in the ruminal milieu and improve nitrogen capture efficiency for microbial biomass synthesis. Enhanced amino acid incorporation can regulate this process [37], and our findings confirm that increased propionate-driven energy availability, combined with direct peptide/amino acid availability, synergistically promoted microbial protein synthesis. The marked elevation of valeric acid content is equally noteworthy. Valerate is both an energy substrate for the host ruminal epithelium and an essential growth factor for obligate cellulolytic bacteria, which require straight- and branched-chain VFAs for cellular lipid synthesis [38]. Concurrent increases in valerate concentration and fiber digestibility strongly support this positive feedback mechanism [39]. Notably, the transient drop in acetic acid content at the intermediate inclusion level (4% inclusion) likely reflects an ecological transition in which the microbiome shifts toward propionate production. As the inclusion percentage increases, robust, multi-pathway functionality is established, elevating overall VFA production without compromising acetogenesis.

4.3. Ruminal and Fecal Microbial Communities and Functional Profiles

Inclusion of 8% FDGs significantly increased the ruminal microbial α-diversity index and induced community-level segregation in β-diversity. Increased α-diversity in ruminal ecosystems is widely recognized as a marker of greater functional redundancy, superior ecological stability, and enhanced capacity to metabolize heterogeneous diets [40]. However, our result contrasts with a cross-species meta-analysis that concluded that fermented feeds generally do not alter ruminal α-diversity in ruminants [41]. This apparent contradiction may be attributable to multi-strain probiotic solid-state fermentation. This process generates postbiotic metabolites to facilitate microbial niche expansion, along with an improved nutritional matrix that supplies nitrogen and lowers selective pressure from recalcitrant fibers [11,42]. β-diversity analysis further highlights that FDGs drive fundamental restructuring of the ruminal microbiome into a highly efficient ecological steady state. The decline in Spirochaetota reflects a reduced reliance on recalcitrant fiber degradation as dietary quality improves, whereas the enrichment of non-photosynthetic Cyanobacteriota aligns with the nitrogen-driven expansion of hemicellulose-degrading and ammonia-assimilating lineages [43]. Furthermore, the expansion of Rikenellaceae_RC9_gut_group provides a direct microbial mechanism explaining the concurrent increase in fiber digestibility and VFA yield [38,44].
Multivariate RDA and Spearman correlation analyses identified six genera with increased relative abundances that were positively associated with ruminal propionic acid, valeric acid, and MCP, including Saccharofermentans and an unclassified genus within Victivallaceae. The enrichment of an unclassified genus within Victivallaceae is particularly noteworthy, as members of this family are fiber-degrading, and acidogenic anaerobes are positively correlated with feed conversion efficiency and volatile fatty acid production [45]. Saccharofermentans is a well-documented carbohydrate-fermenting genus associated with cellulase and xylanase activities, elevated short-chain fatty acid content, and improved feed efficiency in ruminants [46,47,48]. Additional treatment-associated taxa, including Oscillospiraceae g__UCG-004 and Lachnospiraceae g__CAG-196, showed predicted functional associations with polysaccharide degradation and propionate-related fermentation. Novel lineages (e.g., g__Candidatus_Soleaferrea and g__Zag_111) appear to occupy specialized metabolic niches created by postbiotic supplementation [49]. Conversely, the downregulation of less efficient competitors such as Lachnoclostridium and Anaeroplasma indicates that dietary benefits arise from an ecological reconfiguration optimized for energy-rich fermentation [50].
PICRUSt2-based functional predictions indicated that functions associated with the treatment-responsive taxa were significantly enriched in pathways related to protein synthesis and nucleotide, carbohydrate, and amino acid metabolism. The higher predicted representation of purine and pyrimidine metabolism was consistent with the observed increase in MCP concentration, as these pathways supply nucleotides required for RNA and DNA synthesis and microbial biomass formation [36]. Similarly, the higher predicted representation of starch, sucrose, and amino sugar metabolism suggested an increased functional potential for carbohydrate utilization and the generation of substrates relevant to the succinate and acrylate pathways of propionate production [51]. Predicted enrichment of pathways related to alanine, aspartate, glutamate, cysteine, and methionine biosynthesis further suggested altered potential for amino acid assimilation and sulfur metabolism, which may be associated with the high protein content and yeast-derived postbiotics in FDG [52]. However, these PICRUSt2 predictions represent inferred functional potential rather than direct measurements of gene expression, pathway activity, or metabolic flux and therefore require further experimental validation.
In contrast to profound ruminal restructuring, the fecal microbiota response to FDGs was muted, with stable α-diversity and selective enrichment of the phylum Bacillota. This attenuation of dietary treatment effects along the gastrointestinal tract is expected because gastric acid lysis in the abomasum and post-ruminal digestive processes progressively dilute ruminal taxonomic signatures. The selective enrichment of fecal Bacillota reflects the upper-gut expansion of Firmicutes-affiliated fibrolytic taxa, indicating that a subset of these beneficial bacteria survives transit to colonize the hindgut [51,53]. Similar prior findings confirmed that fermented feeds act primarily as targeted ruminal modulators and preserve hindgut microbial homeostasis [14].

4.4. Limitations and Prospects

Although this study established the benefits of FDGs for ruminal health, future research should address some methodological limitations. Firstly, the 28-day experimental trial period was likely too short to generate differences in cumulative growth performance. To better assess FDG effects on this variable, long-term feeding trials across growth stages are needed [30]. Secondly, the rumen fermentation and microbiome analyses included only six samples per treatment, which may have limited statistical power and the generalizability of the findings. Thirdly, functional insights derived from 16S rRNA-inferred PICRUSt2 predictions require direct validation using shotgun metagenomics, metatranscriptomics, and metabolomics. Fourthly, several treatment-associated genera remain uncultivated or poorly characterized; therefore, targeted culturomic isolation and functional validation are needed to clarify their substrate preferences and potential metabolic roles. Finally, incorporating FDG required diet reformulation, resulting in slight differences in ingredient and nutrient composition that may have contributed to the observed responses. Future studies should use isoenergetic and isonitrogenous diets to isolate FDG-specific effects and evaluate the economics of FDG inclusion across diverse basal diets, production systems, and cattle breeds to establish practical feeding recommendations.

5. Conclusions

Dietary inclusion of FDGs on a dry-matter basis optimized ruminal fermentation and fiber utilization in crossbred Simmental steers without adversely affecting overall growth performance or total-tract nutrient digestibility. This nutritional benefit is primarily driven by targeted restructuring of the ruminal microbiome, specifically by enriching key fibrolytic and acidogenic taxa and by upregulating functional pathways involved in nucleotide, carbohydrate, and amino acid metabolism. In summary, 8% FDG produced the greatest response among the inclusion levels tested. FDG promotes energy-efficient, propionate-oriented fermentation and enhances MCP synthesis. This dietary treatment mainly affected the rumen, leaving fecal microbiota diversity and hindgut homeostasis largely intact.

Author Contributions

Methodology, F.C., L.X., Z.W. and C.S.; Formal analysis, F.C., L.X. and H.W.; Investigation, F.C., L.X., Z.W., H.W., Z.T., D.L., C.S., L.M. and W.S.; Conceptualization, Z.T.; Resources, C.S.; Data curation, F.C., L.X., D.L. and W.S.; Visualization, LM; Writing—original draft preparation, F.C. and L.X.; Writing—review and editing, W.S. and Z.S.; Project administration, Z.S.; Supervision, Z.S. All authors have read and agreed to the published version of the manuscript.

Funding

This study was supported by the horizontal commissioned project from Nanjing High Tech Institute of Biotechnology Co., Ltd. (Grant No. F2025820) and the National Natural Science Foundation of China (Grant No. 32673711 and 32272889).

Informed Consent Statement

The Institutional Animal Care and Use Committee of Southwest University approved all animal procedures (IACUC No.: SWU-IACUC-20260123, approved on 2025-08-19).

Data Availability Statement

The raw data for 16S rRNA sequencing are available at NCBI under accession PRJNA1515494 (https://www.ncbi.nlm.nih.gov/bioproject/PRJNA1515494 accwssed on 20 August 2026). The datasets analyzed during the current study are available from the corresponding author upon reasonable request.

Conflicts of Interest

Chuan Song was employed by Luzhou Laojiao Co., Ltd. The remaining authors declare that the research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest. The authors declare that this study received funding from Nanjing High Tech Institute of Biotechnology Co., Ltd. The funder was not involved in the study design, collection, analysis, interpretation of data, the writing of this article, or the decision to submit it for publication.

Appendix A

Table A1. Permutation test results for the redundancy analysis (RDA) model assessing the relationships between core bacterial genera and rumen fermentation parameters (MCP, propionic acid, and valeric acid).
Source of VariationDfVarianceFp
Model30.01132.3210.024
Residual80.0130
Total110.0243
Note: Df, degrees of freedom. The significance of the RDA model was evaluated using 999 Monte Carlo permutations under the reduced model. p < 0.05 indicates statistical significance.

Appendix B

Figure A1. Spearman correlation heatmap between total detected bacterial genera and rumen fermentation parameters. Spearman rank correlation matrix evaluating the relationships between all detected rumen bacterial genera and significantly altered fermentation parameters (MCP, propionic acid, and valeric acid). Color scale represents the Spearman correlation coefficient, ranging from blue (negative correlation) to red (positive correlation). Asterisks denote statistical significance (* p < 0.05, ** p < 0.01, *** p < 0.001). Abbreviations: MCP, microbial protein.
Agriculture 16 02131 g0a1

Appendix C

Table A2. Detailed functional annotations of the 30 selected KEGG Orthology terms presented in the genus–KO heatmap.
KODescription
ko:K03091sigE_F_G; RNA polymerase sigma-E/F/G factor
ko:K07133K07133; uncharacterized protein
ko:K21071pfk, pfp; ATP-dependent phosphofructokinase / diphosphate-dependent phosphofructokinase [EC:2.7.1.11 2.7.1.90]
ko:K03654recQ; ATP-dependent DNA helicase RecQ [EC:5.6.2.4]
ko:K02015ABC.FEV.P; iron complex transport system permease protein
ko:K10536aguA; agmatine deiminase [EC:3.5.3.12]
ko:K02013ABC.FEV.A; iron complex transport system ATP-binding protein [EC:7.2.2.-]
ko:K01992ABC-2.P; ABC-2 type transport system permease protein
ko:K02027ABC.MS.S; multiple sugar transport system substrate-binding protein
ko:K06142hlpA, ompH; outer membrane protein
ko:K03665hflX; GTPase
ko:K04068nrdG; anaerobic ribonucleoside-triphosphate reductase activating protein [EC:1.97.1.4]
ko:K17320lplC; putative aldouronate transport system permease protein
ko:K06158ABCF3; ATP-binding cassette, subfamily F, member 3
ko:K17319lplB; putative aldouronate transport system permease protein
ko:K13653K13653; AraC family transcriptional regulator
ko:K03704cspA; cold shock protein
ko:K07718yesM; two-component system, sensor histidine kinase YesM [EC:2.7.13.3]
ko:K15738uup; ABC transport system ATP-binding/permease protein
ko:K03088rpoE; RNA polymerase sigma-70 factor, ECF subfamily
ko:K07636phoR; two-component system, OmpR family, phosphate regulon sensor histidine kinase PhoR [EC:2.7.13.3]
ko:K02014TC.FEV.OM; iron complex outermembrane recepter protein
ko:K03437spoU; RNA methyltransferase, TrmH family
ko:K03169topB; DNA topoisomerase III [EC:5.6.2.1]
ko:K01921ddl; D-alanine-D-alanine ligase [EC:6.3.2.4]
ko:K03797E3.4.21.102, prc, ctpA; carboxyl-terminal processing protease [EC:3.4.21.102]
ko:K02004ABC.CD.P; putative ABC transport system permease protein
ko:K03406mcp; methyl-accepting chemotaxis protein
ko:K01990ABC-2.A; ABC-2 type transport system ATP-binding protein
ko:K02016ABC.FEV.S; iron complex transport system substrate-binding protein

References

  1. Sun, X.; Dou, Z.X.; Shurson, G.C.; Hu, B. Bioprocessing to upcycle agro-industrial and food wastes into high-nutritional value animal feed. Resour. Conserv. Recycl. 2024, 201, 107325. [Google Scholar] [CrossRef] [Scilit]
  2. Greenwood, P.L. Review: An overview of beef production from pasture and feedlot globally, as demand for beef and the need for sustainable practices increase. Animal 2021, 15, 100295. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Yafetto, L.; Odamtten, G.T.; Wiafe-Kwagyan, M. Valorization of agro-industrial wastes into animal feed through microbial fermentation: A review of the global and Ghanaian case. Heliyon 2023, 9, e14814. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Dhiman, S.; Kumar, A.; Sharma, K.; Dhewa, T. Microbial Bioprocessing of Food and Agro-Industrial Residues for a Sustainable Circular Economy. Indian J. Microbiol. 2025, 65, 1452–1483. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Liu, Y.; Liu, S.; Huang, C.; Ge, X.; Xi, B.; Mao, J. Chinese Baijiu distiller’s grains resourcing: Current progress and future prospects. Resour. Conserv. Recycl. 2022, 176, 105900. [Google Scholar] [CrossRef] [Scilit]
  6. Virgínio Júnior, G.F.; Loregian, K.E.; Millen, D.D. Distillers’ grains as alternative feed resources for beef cattle: Review. Anim. Biosci. 2026, 39, 250771. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Buenavista, R.M.E.; Siliveru, K.; Zheng, Y. Utilization of Distiller’s dried grains with solubles: A review. J. Agric. Food Res. 2021, 5, 100195. [Google Scholar] [CrossRef] [Scilit]
  8. Liu, J.; Wang, S.; Wang, Z.; Shen, C.; Liu, D.; Shen, X.; Weng, L.; He, Y.; Wang, S.; Wang, J.; et al. Pretreatment of Luzhou distiller’s grains for feed protein production using crude enzymes produced by a synthetic microbial consortium. Bioresour. Technol. 2023, 390, 129852. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Plaizier, J.C.; Mulligan, F.J.; Neville, E.W.; Guan, L.L.; Steele, M.A.; Penner, G.B. Invited review: Effect of subacute ruminal acidosis on gut health of dairy cows. J. Dairy Sci. 2022, 105, 7141–7160. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Murtaza, B.; Ling-ling, G.; Wang, L.; Li, X.; Ali, A.; Saleemi, M.K.; Khatoon, A.; Haq, S.U.; Jin, B.; Li, J.-b.; et al. Mycotoxin detection in corn and distillers dried grains for food security. Renew. Sustain. Energy Rev. 2025, 210, 115194. [Google Scholar] [CrossRef] [Scilit]
  11. Yang, L.; Zhang, J.; Chen, Z.; Chen, Y.; Wang, C.; Yu, H.; Zuo, F.; Huang, W. Probiotic-Enzyme Synergy Regulates Fermentation of Distiller’s Grains by Modifying Microbiome Structures and Symbiotic Relationships. J. Agric. Food Chem. 2025, 73, 5363–5375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Zhang, S.; Huang, Z.; Li, Q.; Zheng, X.; Liu, J. Two-stage solid-state fermentation to increase the nutrient value of corn processing waste and explore its efficacy as a feed protein source. Food Chem. X 2024, 23, 101656. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Zhang, R.; Mei, S.; He, G.; Wei, M.; Chen, L.; Chen, Z.; Zhong, Y.; Zhou, B.; Wang, K.; Cheng, Z.; et al. Feeding probiotics-fermented distiller’s grains diets increases rumen enzyme activities and glycerophospholipid levels in finishing cattle by modulating rumen microbiota. Microbiome 2025, 13, 137. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Zhang, R.; Mei, S.; He, G.; Wei, M.; Chen, L.; Chen, Z.; Zhu, M.; Zhou, B.; Wang, K.; Cheng, Z.; et al. Multi-omics analyses reveal fecal microbial community and metabolic alterations in finishing cattle fed probiotics-fermented distiller’s grains diets. Microbiol. Spectr. 2025, 13, e0072124. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Mei, S.; He, G.; Zhang, T.; Chen, Z.; Zhang, R.; Liao, Y.; Zhu, M.; Xu, D.; Shen, Y.; Zhou, B.; et al. Effect of feeding fermented distiller’s grains diets on immune status and metabolomics of spleen and mesenteric lymph nodes in finishing cattle. J. Proteom. 2024, 296, 105107. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. NY/T 815-2004; National Research Council (NRC). Nutrient Requirements of Beef Cattle. The National Academies Press: Washington, DC, USA, 2004.
  17. NY/T 815-2004; Feeding Standard of Beef Cattle. China Agriculture Press: Beijing, China, 2004.
  18. Chaney, A.L.; Marbach, E.P. Modified reagents for determination of urea and ammonia. Clin. Chem. 1962, 8, 130–132. [Google Scholar] [CrossRef] [Scilit]
  19. Broderick, G.A.; Kang, J.H. Automated simultaneous determination of ammonia and total amino acids in ruminal fluid and in vitro media. J. Dairy Sci. 1980, 63, 64–75. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Bradford, M.M. A rapid and sensitive method for the quantitation of microgram quantities of protein utilizing the principle of protein-dye binding. Anal. Biochem. 1976, 72, 248–254. [Google Scholar] [CrossRef] [PubMed]
  21. Erwin, E.S.; Marco, G.J.; Emery, E.M. Volatile fatty acid analyses of blood and rumen fluid by gas chromatography. J. Dairy Sci. 1961, 44, 1768–1771. [Google Scholar] [CrossRef] [Scilit]
  22. Foote, A.P. TECHNICAL NOTE: Analysis of volatile fatty acids in rumen fluid by gas chromatography mass spectrometry using a dimethyl carbonate extraction. J. Anim. Sci. 2022, 100, skac207. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. GB/T 6432-2018; Determination of crude protein in feeds—Kjeldahl method. Standards Press of China: Beijing, China, 2018.
  24. GB/T 20806-2022; Determination of neutral detergent fiber (NDF) in feeds. Standards Press of China: Beijing, China, 2022.
  25. NY/T 1459-2022; Determination of acid detergent fiber (ADF) in feeds. China Agriculture Press: Beijing, China, 2022.
  26. GB/T 6436-2018; Determination of calcium in feeds. Standards Press of China: Beijing, China, 2018.
  27. GB/T 6437-2018; Determination of phosphorus in feeds. Standards Press of China: Beijing, China, 2018.
  28. GB/T 6438-2007; Animal feeding stuffs—Determination of crude ash. Standards Press of China: Beijing, China, 2007.
  29. Castillo-Lopez, E.; Ricci, S.; Rivera-Chacon, R.; Sener-Aydemir, A.; Pacífico, C.; Reisinger, N.; Schwartz-Zimmermann, H.E.; Berthiller, F.; Kreuzer-Redmer, S.; Zebeli, Q. Dynamic interplay of immune response, metabolome, and microbiota in cows during high-grain feeding: Insights from multi-omics analysis. Microbiol. Spectr. 2024, 12, e0094424. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Wang, Z.; Li, Y.; Tang, H.; Luo, D.; Huang, J.; Ye, B.; Yan, W.; Liu, G.; Yang, Y. Novel fermentation strategy utilizing a probiotic complex to improve the feeding value of distillers’ grains. Ind. Crops Prod. 2025, 226, 120748. [Google Scholar] [CrossRef] [Scilit]
  31. Firkins, J.L.; Henderson, E.L.; Duan, H.; Pope, P.B. International Symposium on Ruminant Physiology: Current perspective on rumen microbial ecology to improve fiber digestibility. J. Dairy Sci. 2025, 108, 7511–7529. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Lai, A.; Huang, Y.; Luo, H.; Jin, Y.; Wang, L.; Chen, B.; Deng, K.; Huang, W.; Zhang, Y. Ruminal degradation characteristics of bagasse with different fermentation treatments in the rumen of beef cattle. Anim. Sci. J. 2024, 95, e13937. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Kaur, H.; Kaur, G.; Gupta, T.; Mittal, D.; Ali, S.A. Integrating Omics Technologies for a Comprehensive Understanding of the Microbiome and Its Impact on Cattle Production. Biology 2023, 12, 1200. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Ye, X.; Sahana, G.; Lund, M.S.; Cai, Z. The crosstalk between host and rumen microbiome in cattle: Insights from multi-omics approaches and genome-wide association studies. World J. Microbiol. Biotechnol. 2025, 41, 267. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Pang, R.; Xiao, X.; Mao, T.T.; Yu, J.J.; Huang, L.; Xu, W.; Li, Y.; Zhu, W. The molecular mechanism of propionate-regulating gluconeogenesis in bovine hepatocytes. Anim. Biosci. 2023, 36, 1693–1699. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Dong, C.; Wei, M.; Ju, J.; Du, L.; Zhang, R.; Xiao, M.; Zheng, Y.; Bao, H.; Bao, M. Effects of guanidinoacetic acid on in vitro rumen fermentation and microflora structure and predicted gene function. Front. Microbiol. 2024, 14, 1285466. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Shan, Q.; Ma, F.; Huang, Q.; Wo, Y.; Sun, P. Chromium yeast promotes milk protein synthesis by regulating ruminal microbiota and amino acid metabolites in heat-stressed dairy cows. Anim. Nutr. 2024, 20, 120–130. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Yu, S.; Li, L.; Zhao, H.; Tu, Y.; Liu, M.; Jiang, L.; Zhao, Y. Characterization of the Dynamic Changes of Ruminal Microbiota Colonizing Citrus Pomace Waste during Rumen Incubation for Volatile Fatty Acid Production. Microbiol. Spectr. 2023, 11, e0351722. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Beckett, L.; Gleason, C.B.; Bedford, A.; Liebe, D.; Yohe, T.T.; Hall, M.B.; Daniels, K.M.; White, R.R. Rumen volatile fatty acid molar proportions, rumen epithelial gene expression, and blood metabolite concentration responses to ruminally degradable starch and fiber supplies. J. Dairy Sci. 2021, 104, 8857–8869. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. Costa-Roura, S.; Villalba, D.; Balcells, J.; De la Fuente, G. First Steps into Ruminal Microbiota Robustness. Animals 2022, 12, 2366. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  41. Khiaosa-Ard, R.; Pacífico, C.; Mahmood, M.; Mickdam, E.; Meixner, J.; Traintinger, L.S.; Zebeli, Q. Changes in the solid-associated bacterial and fungal communities following ruminal in vitro fermentation of winery by-products: Aspects of the bioactive compounds and feed safety. Anaerobe 2024, 89, 102893. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Zhong, J.; Zhou, D.; Hu, P.; Cheng, Y.; Huang, Y. Identification of the chemical composition of distiller’s grain polyphenols and their effects on the fecal microbial community structure. Food Chem. X 2023, 20, 101001. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Martinez-Fernandez, G.; Jiao, J.; Padmanabha, J.; Denman, S.E.; McSweeney, C.S. Seasonal and Nutrient Supplement Responses in Rumen Microbiota Structure and Metabolites of Tropical Rangeland Cattle. Microorganisms 2020, 8, 1550. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  44. Peng, W.; Wang, Y.; Wei, M.; Liu, S.; Liu, K.; Xiao, M.; Zhang, R.; Wang, Y.; Zheng, Y.; Fang, L.; et al. Effects of changes in rumen microbial adaptability on rumen fermentation and nutrient digestion in Horqin beef cattle during different seasons of grazing and supplementary feeding. BMC Microbiol. 2025, 25, 556. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Kim, H.; Park, T.; Kwon, I.; Seo, J. Specific inhibition of Streptococcus bovis by endolysin LyJH307 supplementation shifts the rumen microbiota and metabolic pathways related to carbohydrate metabolism. J. Anim. Sci. Biotechnol. 2021, 12, 93. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Hu, Y.; He, Y.; Gao, S.; Liao, Z.; Lai, T.; Zhou, H.; Chen, Q.; Li, L.; Gao, H.; Lu, W. The effect of a diet based on rice straw co-fermented with probiotics and enzymes versus a fresh corn Stover-based diet on the rumen bacterial community and metabolites of beef cattle. Sci. Rep. 2020, 10, 10721. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Zhang, Y.K.; Zhang, X.X.; Li, F.D.; Li, C.; Li, G.Z.; Zhang, D.Y.; Song, Q.Z.; Li, X.L.; Zhao, Y.; Wang, W.M. Characterization of the rumen microbiota and its relationship with residual feed intake in sheep. Animal 2021, 15, 100161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  48. Rabee, A.E.; Younan, B.R.; Kewan, K.Z.; Sabra, E.A.; Lamara, M. Modulation of rumen bacterial community and feed utilization in camel and sheep using combined supplementation of live yeast and microalgae. Sci. Rep. 2022, 12, 12990. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  49. Xie, Y.Y.; Sun, H.Z.; Xue, M.Y.; Liu, J.X. Metagenomics reveals differences in microbial composition and metabolic functions in the rumen of dairy cows with different residual feed intake. Anim. Microbiome 2022, 4, 19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Li, C.; Chen, N.; Zhang, X.; Shahzad, K.; Qi, R.; Zhang, Z.; Lu, Z.; Lu, Y.; Yu, X.; Zafar, M.H.; et al. Mixed silage with Chinese cabbage waste enhances antioxidant ability by increasing ascorbate and aldarate metabolism through rumen Prevotellaceae UCG-004 in Hu sheep. Front. Microbiol. 2022, 13, 978940. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  51. Ricci, S.; Pacifico, C.; Castillo-Lopez, E.; Rivera-Chacon, R.; Schwartz-Zimmermann, H.E.; Reisinger, N.; Berthiller, F.; Zebeli, Q.; Petri, R.M. Progressive microbial adaptation of the bovine rumen and hindgut in response to a step-wise increase in dietary starch and the influence of phytogenic supplementation. Front. Microbiol. 2022, 13, 920427. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  52. Guo, J.; Zhang, Z.; Guan, L.L.; Yoon, I.; Plaizier, J.C.; Khafipour, E. Postbiotics from Saccharomyces cerevisiae fermentation stabilize microbiota in rumen liquid digesta during grain-based subacute ruminal acidosis (SARA) in lactating dairy cows. J. Anim. Sci. Biotechnol. 2024, 15, 101. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  53. Khatoon, M.; Patel, S.H.; Pandit, R.J.; Jakhesara, S.J.; Rank, D.N.; Joshi, C.G.; Kunjadiya, A.P. Rumen and fecal microbial profiles in cattle fed high lignin diets using metagenome analysis. Anaerobe 2022, 73, 102508. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Table 1. Nutritional composition of distillers’ grains before and after fermentation (Dry matter basis, %).
ItemsBefore FermentationAfter Fermentation
CP16.7734.14
TP13.5020.09
NDF60.8231.37
ADF49.1922.66
Ash10.3612.24
P0.260.50
Ca0.120.74
Abbreviations: CP, crude protein; TP, true protein; NDF, neutral detergent fiber; ADF, acid detergent fiber; P, phosphorus; Ca, calcium.
Table 2. Ingredients and nutritional composition of experimental diets (Dry matter basis, %).
ItemsTreatments (1)
Control4% Group8% Group
Ingredients
Corn22.3323.3323.33
Soybean meal2.232.232.23
Concentrate (2)8.928.928.92
Ordinary distiller’s grains38.4634.4629.50
Fermented distiller’s grains 4.008.00
Wheat straw26.9225.9226.88
Bicarbonate of soda1.121.121.12
Mycotoxin binder0.020.020.02
Total100.00100.00100.00
Chemical composition
NEm/(Mcal/kg) (3)1.551.561.56
NEg/(Mcal/kg) (3)0.910.920.92
NEmf/(Mcal/kg) (3)2.462.482.48
CP13.5113.7914.05
NDF36.0435.3835.60
ADF20.6120.3520.61
P0.340.340.34
Ca0.550.550.55
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains. (2) Concentrate: On a dry matter basis, the concentrate feed provides per kilogram of diet: 26.76 g soybean meal, 31.22 g cottonseed and rapeseed meal, 13.38 g limestone, 5.35 g salt, 3.57 g dicalcium phosphate, 2.68 g urea, and 6.24 g compound premix. This contributes 32.6 g (3.26%) crude protein, 5.5 g (0.55%) calcium, 0.9 g (0.09%) phosphorus, and 5.4 g (0.54%) salt per kilogram of total diet. (3) The net energy is calculated in accordance with NY/T 815-2004 [17]; the remaining values are measured values. Abbreviations: NEm, net energy for maintenance; NEg, net energy for gain; NEmf, comprehensive net energy; CP, crude protein; NDF, neutral detergent fiber; ADF, acid detergent fiber; P, phosphorus; Ca, calcium.
Table 3. Effects of different proportions of fermented distiller’s grains on the growth performance of crossbred steers.
ItemsTreatments (1)SEMp-Value
Control4% Group8% GroupTreatmentLinearQuadratic
IBW/kg343.96336.96334.963.4310.545--
FBW/kg380.21374.58374.004.7870.850--
ADG/(kg/d)1.301.341.390.0700.846--
DMI/(kg/d)9.839.649.590.1410.718--
F/G8.318.027.890.5410.780--
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains (n = 12). Data are presented as mean and SEM, with p < 0.05 indicating statistical significance. Abbreviations: IBW, initial body weight; FBW, final body weight; ADG, average daily gain; DMI, dry matter intake; F/G, feed-to-gain ratio.
Table 4. Effect of different proportions of fermented distiller’s grains on the apparent digestibility in crossbred steers (%).
ItemsTreatments (1)SEMp-Value
Control4% Group8% GroupTreatmentLinearQuadratic
DM74.9775.1675.340.4150.943--
CP69.9670.1469.880.4430.974--
NDF63.10 b63.20 b65.45 a0.4200.0240.9150.007
ADF52.9354.3555.730.7840.368--
P51.2251.3852.960.8550.682--
Ca51.2850.2949.950.9660.858--
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains (n = 6). Data are presented as mean and SEM, with p < 0.05 indicating statistical significance. a, b indicate that differences among the same letters are not significant, while differences among different letters are significant. Abbreviations: DM, dry matter; CP, crude protein; NDF, neutral detergent fiber; ADF, acid detergent fiber; P, phosphorus; Ca, calcium.
Table 5. Effects of different addition ratios of fermented distillers’ grains on rumen fermentation parameters in cross-bred steers.
ItemsTreatments (1)SEMp-Value
Control4% Group8% GroupTreatmentLinearQuadratic
NH4-N/(mg/dL)16.4515.6516.750.4960.671--
MCP/(mg/mL)0.54 b0.75 ab0.82 a0.0470.0300.0510.054
pH6.796.836.850.0160.477--
AA/(g/L)3.76 a3.58 b3.76 a0.0320.0160.0120.103
PA/(g/L)1.47 b1.50 ab1.53 a0.0090.0330.11950.019
BA/(g/L)1.231.201.250.0100.140--
IBA/(g/L)0.120.100.110.0040.050--
VA/(g/L)0.153 b0.173 a0.173 a0.0030.0040.0040.065
IVA/(g/L)0.200.210.210.0040.381--
A/P2.56 a2.39 b2.46 ab0.0260.0180.0050.821
TVFA/(g/L)6.93 ab6.75 b7.03 a0.0460.038--
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains (n = 6). Data are presented as mean and SEM, with p < 0.05 indicating statistical significance. a, b indicate that differences among the same letters are not significant, while differences among different letters are significant. Abbreviations: NH3-N, ammonia nitrogen; MCP, microbial protein; AA, acetic acid; PA, propionic acid; BA, butyric acid; IBA, isobutyric acid; VA, valeric acid; IVA, isovaleric acid; A/P, ratio of acetic to propionic acid; TVFA, total volatile fatty acids.
Table 6. Effect of different proportions of fermented distiller’s grains on the rumen microbial community abundance in cross-bred steers (%).
ItemsTreatments (1)SEMp-Value
Control4% Group8% Group
Phylum level
Bacteroidota63.9961.1261.521.2120.607
Bacillota30.1631.9231.211.2940.869
Pseudomonadota1.812.252.250.1500.359
Verrucomicrobiota1.031.661.740.1590.141
Spirochaetota1.41 a1.18 ab0.89 b0.0770.013
Cyanobacteriota0.37 b0.52 ab0.98 a0.1040.029
Patescibacteria0.430.550.550.0240.062
Fibrobacterota0.400.340.360.0230.561
Actinomycetota0.160.200.220.0200.510
Elusimicrobiota0.050.050.040.0050.687
Genus level
Xylanibacter43.4138.4535.751.4300.077
Rikenellaceae RC9 gut group4.45 b5.53 b6.72 a0.2860.001
Ruminococcus5.846.636.750.3890.614
Bacteroidales RF16 group4.184.836.190.3900.091
Clostridia UCG-0143.02 a2.79 ab2.29 b0.1280.049
Christensenellaceae R-7 group1.201.371.500.1040.523
Eubacterium coprostanoligenes group1.011.151.240.0480.150
UCG-0100.840.940.910.0310.360
UCG-0050.440.430.400.0280.867
Unclassified Lachnospiraceae0.380.440.410.0230.522
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains (n = 6). Data are presented as mean and SEM, with p < 0.05 indicating statistical significance. a, b indicate that differences among the same letters are not significant, while differences among different letters are significant.
Table 7. Effect of different proportions of fermented distiller’s grains on the microbial community abundance in the feces of cross-bred steers (%).
ItemsTreatments(1)SEMp-Value
Control4% Group8% Group
Phylum level
Bacillota67.83 b76.39 a76.69 a1.6040.026
Bacteroidota24.5819.3318.351.4030.150
Spirochaetota4.782.372.780.7830.567
Pseudomonadota1.460.210.200.3880.144
Verrucomicrobiota0.620.530.430.0880.700
Cyanobacteriota0.300.490.570.0550.111
Patescibacteria0.220.240.470.0600.176
Actinomycetota0.110.280.450.0700.054
Elusimicrobiota0.040.090.020.0220.640
Fibrobacterota<0.01<0.01<0.01<0.0010.368
Genus level
Clostridia UCG-01413.5212.2211.550.5180.303
Ruminococcus5.238.347.750.8110.265
Rikenellaceae RC9 gut group9.636.296.800.6170.050
Christensenellaceae R-7 group5.085.615.660.2840.681
Bacteroidales RF16 group5.595.305.510.2920.928
Unclassified Lachnospiraceae4.683.835.360.2730.064
Eubacterium coprostanoligenes group3.833.451.630.5220.080
UCG-0100.680.540.660.0870.806
Xylanibacter<0.010.02<0.010.0030.090
(1) Control: diet formulated without fermented distillers’ grains; 4% group: diet formulated to contain 4% fermented distillers’ grains; 8% group: diet formulated to contain 8% fermented distillers’ grains (n = 6). Data are presented as mean and SEM, with p < 0.05 indicating statistical significance. a, b indicate that differences among the same letters are not significant, while differences among different letters are significant.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.