Article

Biofertilization with Gluconacetobacter diazotrophicus: Effects of a Native Isolate and a Reference Strain on Soil and Foliar Chemical Profiles and Economic Performance in Greenhouse Tomato Production

by
Nelson Ceballos-Aguirre
1,
Gloria M. Restrepo
2,
Alejandro Hurtado-Salazar
1,
Mariana Pachón
2,
Jorge A. Cuéllar
2 and
Óscar J. Sánchez
3,*
1
Faculty of Agricultural Sciences, Universidad de Caldas, Calle 65 No. 26-10, Manizales 170004, Colombia
2
Research Institute in Microbiology and Agro-Industrial Biotechnology, Universidad Católica de Manizales, Carrera 23 No. 60-63, Manizales 170002, Colombia
3
Center for Technological Development—Bioprocess and Agro-Industry Plant, Department of Engineering, Universidad de Caldas, Calle 65 No. 26-10, Manizales 170004, Colombia
*
Author to whom correspondence should be addressed.
Agriculture 2026, 16(14), 1493; https://doi.org/10.3390/agriculture16141493
Submission received: 8 May 2026 / Revised: 30 June 2026 / Accepted: 7 July 2026 / Published: 9 July 2026

Abstract

The intensive use of synthetic fertilizers in horticulture generates environmental and economic constraints, highlighting the need for sustainable alternatives such as plant growth-promoting bacteria. However, their effectiveness depends on strain adaptation to local conditions. This study evaluated the effect of Gluconacetobacter diazotrophicus (native isolate GIBI029 vs. reference strain ATCC 49037) under four nitrogen (0 and 100% of the recommended dose) and phosphorus (0 and 100% of the recommended dose) fertilization combinations on soil chemical properties, foliar nutrient uptake, and economic performance in greenhouse tomato production in Colombia. The native isolate was associated with higher soil nutrient levels, reaching 185.1 g/kg organic matter, 6.4 g/kg total nitrogen, 284.75 mg/kg available phosphorus, 9.32 cmol/kg calcium, and 3.93 cmol/kg magnesium. In addition, foliar nitrogen content reached 22.4 g/kg in treatments inoculated with GIBI029. These responses were associated with yields up to 106.4 t/ha, exceeding those obtained with the reference strain. Yield data were obtained from a previous study conducted under the same experimental design and environmental conditions and were incorporated here exclusively for the economic assessment. Economically, the native isolate achieved the highest benefit–cost ratio (2.65) and net income (USD 20,106/ha). A strong correlation between soil organic matter and nitrogen (r = 0.99) was observed, indicating a close association between these variables within the evaluated production system. These results suggest that strain origin may influence biofertilization efficiency and indicate that native microbial inoculants can contribute to improved agronomic and economic performance under the conditions evaluated, supporting their use in sustainable tomato production systems.

1. Introduction

Tomato (Solanum lycopersicum L.) production under protected conditions still depends strongly on synthetic fertilization, particularly nitrogen (N) and phosphorus (P). This dependence increases production costs and contributes to environmental pressure. Therefore, biofertilization with plant growth-promoting rhizobacteria (PGPR) has gained attention as a strategy to improve nutrient-use efficiency and support more sustainable production systems. The value of these microorganisms is not limited to general growth promotion. It also depends on their capacity to influence nutrient acquisition, rhizosphere processes, and crop performance under specific production conditions [1,2,3,4].
The effectiveness of microbial inoculants is strongly context-dependent. Inoculated microorganisms do not act in isolation, and their performance depends on root colonization, interactions with the resident microbiota, soil nutrient status, and crop management. Therefore, strain identity may be a key agronomic factor rather than a minor microbiological feature [3,4,5].
These considerations are particularly relevant for diazotrophic bacteria. Among them, Gluconacetobacter diazotrophicus is one of the best-known endophytic bacteria associated with plant–microbe interactions in non-leguminous crops. This species was first isolated from sugarcane by Cavalcante and Döbereiner [6]. More recent studies have shown that its performance is functionally specific. Gene fitness during diazotrophic growth depends on particular genetic determinants, and ammonium release can be modified experimentally. These findings indicate that strain performance should not be inferred from taxonomy alone [7,8].
The agronomic role of G. diazotrophicus is not restricted to N. In strawberry, this bacterium improved P nutrition under P deficiency and contributed to iron acquisition through siderophore-related mechanisms. These findings suggest that its effects may involve several nutrient-related pathways [9,10].
In tomato, however, the available evidence remains limited and, in some cases, fragmented. Open-field studies have shown that inoculation with G. diazotrophicus can reduce N fertilizer requirements without affecting fruit quality [11]. At early growth stages, plant responses depend on genotype, bacterial dose, and P availability [12]. In Colombia, native isolates from local production systems have shown plant growth-promoting traits, including phosphate solubilization, indole-compound production, and nitrogenase activity [13].
Under protected cultivation, the use of G. diazotrophicus has also been associated with improvements in several technical and economic indicators [14]. In addition, a recent study conducted under the same experimental framework as the present work showed that the native isolate GIBI029 maintained high tomato yield under contrasting N and P fertilization regimes. This result suggested an important role of strain origin and local adaptation [15].
Recent studies with other PGPR in tomato have also broadened the agronomic context in which microbial inoculation should be evaluated. Improvements in plant growth, P availability, soil quality, and yield have been reported with Pseudomonas putida [16], phosphorus-solubilizing bacteria [17], Bacillus subtilis [18], and native rhizobia [19]. However, the magnitude and direction of these responses vary according to crop stage, soil conditions, and inoculant type. Similar responses have been observed in pepper [20], lettuce [21], and pak choi [22], where PGPR increased soil nutrient availability, plant nutrient concentration, or crop productivity. In cucumber, however, bacterial inoculation depends strongly on nutrient availability and may alter mineral composition in different ways [23]. These findings confirm that PGPR responses are system-specific.
Despite these advances, most studies still evaluate only one part of the crop response. Soil measurements, foliar composition, yield, and profitability are often reported separately. This approach makes it difficult to determine whether changes in soil nutrient status are associated with plant nutrient uptake and economic performance. This limitation is particularly relevant in greenhouse systems, where high input costs require a more integrated interpretation of microbial inoculation.
The agronomic value of PGPR is better understood when they are evaluated in terms of soil nutrient availability, plant uptake, crop performance, and profitability. However, this integrated perspective has rarely been applied to G. diazotrophicus in greenhouse tomato production. Most previous studies have focused on isolated variables, such as biomass, yield, or fertilizer substitution. Less information is available on whether inoculation is associated with changes in residual soil chemical properties and foliar nutrient status within the same production system.
This knowledge gap is especially relevant for native isolates. A locally adapted isolate may perform differently from a reference strain, even within the same bacterial species. This difference may result from greater compatibility with the host plant, soil environment, and fertilization regime. In the present case, previous studies identified GIBI029 as a Colombian native isolate of G. diazotrophicus with stronger plant growth-promoting traits than the reference strain ATCC 49037. This same isolate also showed superior yield performance under the same basic experimental conditions [13,15].
Nevertheless, those studies did not integrate residual soil chemistry, foliar nutrient composition, and economic response in a single analysis. Therefore, the central question addressed here is whether the native isolate GIBI029 is associated with a distinct soil and foliar chemical profile that helps explain its agronomic and economic value in greenhouse tomato production. This approach also helps determine whether the advantage of the native isolate is expressed only in yield or also in the chemical profile of the production system.
Previous evidence shows that the native isolate GIBI029 can improve agronomic performance in greenhouse tomato production. Based on this, we formulated the following hypotheses: (i) GIBI029 would improve soil and foliar chemical profiles more effectively than the reference strain ATCC 49037 and the non-inoculated control treatments; (ii) these changes would be associated with differences in soil and foliar nutrient profiles; and (iii) the improved agronomic response would translate into superior economic performance under greenhouse tomato production conditions.
Therefore, the objective of this study was to evaluate the effect of G. diazotrophicus, comparing the native Colombian isolate GIBI029 with the reference strain ATCC 49037, on soil and foliar chemical profiles and on the economic feasibility of its use in greenhouse tomato production. An important contribution of this study is the integration of new soil and foliar nutrient data with previously validated yield data obtained under the same experimental conditions. This integrated approach provides a more complete agronomic and economic assessment of microbial inoculation and allows strain origin to be interpreted in relation to nutrient dynamics, crop performance, and production profitability.

2. Materials and Methods

2.1. Location

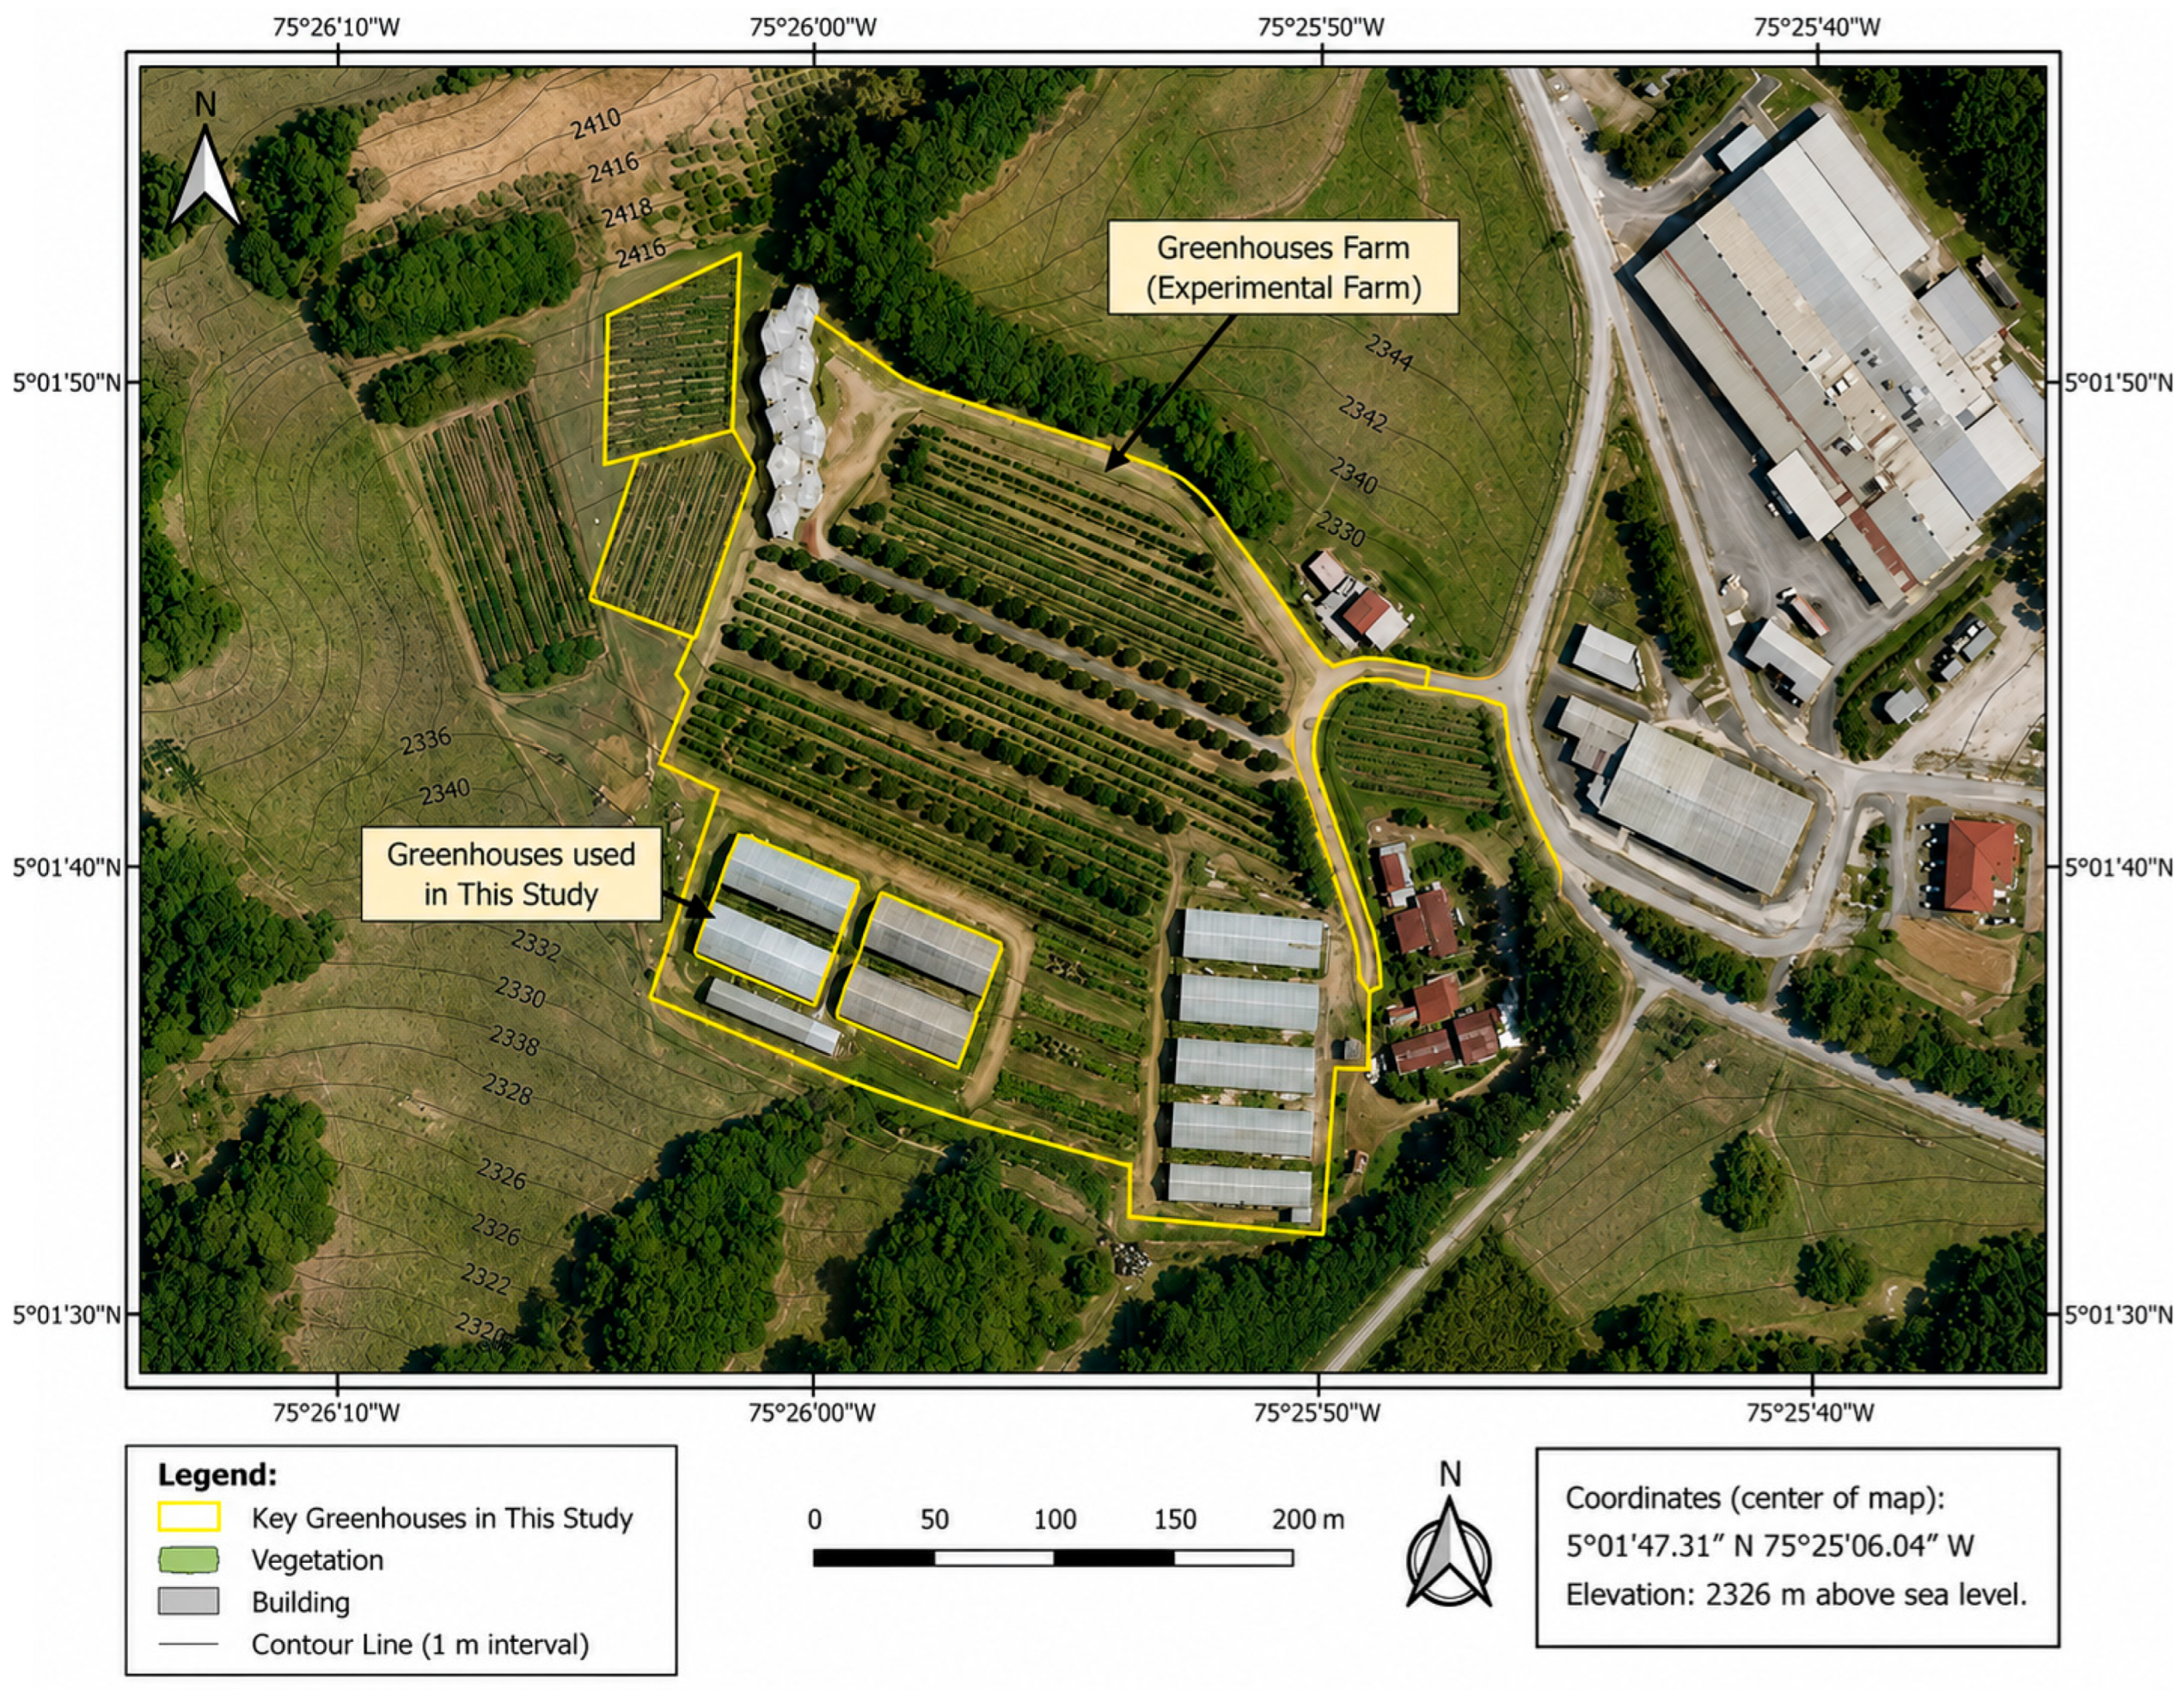
This study was conducted at the Tesorito farm of the University of Caldas, Manizales, Colombia (5°01′47.31″ N and 75°26′06.04″ W, 2326 m above sea level, see Figure 1), with an annual rainfall of 1800 mm, relative humidity of 78%, and a mean temperature of 17.5 °C [24].
The site’s soil corresponds to volcanic ash-derived Andisols characterized by allophanic materials. Previous soil surveys classified the dominant soil unit as Typic Udivitrands according to USDA Soil Taxonomy. Based on the correlation with the World Reference Base for Soil Resources, these soils correspond to Vitric Andosols according to the International Union of Soil Sciences classification system [25]. The volcanic origin, high content of glassy materials, and humid climatic conditions of the study area support this classification. Field experiments were conducted at the Tesorito farm from January to August 2022.

2.2. Plant Material and Bacteria

A commercial Chonto-type tomato hybrid (Roble 956 F1 Hybrid Tomato; ImpulSemillas, Tocancipá, Colombia) was used in this study. This hybrid exhibits indeterminate growth, strong stems, medium internodes, and an average fruit weight ranging from 140 to 160 g. According to the manufacturer’s technical specifications, it is adapted to production areas with cold to moderate climatic conditions at elevations between 1800 and 2200 m a.s.l., where average temperatures range from 17 to 20 °C. In addition, it shows tolerance to low temperatures and resistance to nematodes, Tomato Mosaic Virus, and Fusarium wilt races 1, 2, and 3 [26]. Certified seeds were obtained from ImpulSemillas and are registered and authorized for commercial distribution by the Colombian Agricultural Institute (ICA, Bogotá, Colombia) under the commercial name “Tomate Híbrido Roble” [27]. During the seedling phase, irrigation, fertilization, and integrated pest and disease management were carried out according to the recommendations of Jaramillo et al. [28].
Tomato seeds were sown in 128-cell nursery trays previously disinfected with a 5 mL/L solution of Agrodyne® (West, La Estrella, Colombia) and sun-dried. The trays were filled with grade 4 peat-type substrate, ensuring no compaction, with seeds placed at a depth twice their size. Seedlings were cultivated under semi-controlled conditions for approximately 30 days. Once the plants reached the four-true-leaf stage, including standard irrigation and pest management protocols, they were deemed ready for transplanting [15].
Two microorganisms were used: the commercial reference strain G. diazotrophicus PAL-5 (ATCC 49037), acquired from the American Type Culture Collection (Manassas, VA, USA), and the Colombian native GIBI029 isolate from Caldas region, provided by the Institute of Microbiology and Agro-Industrial Biotechnology of the Universidad Católica de Manizales (Manizales, Colombia). The methodology for the production of the bacterial suspension is described in previous work [29].

2.3. Experimental Design

The experiment was conducted in a split-plot design with four replications per treatment and 10 plants as the experimental unit. The main plot consisted of the reference strain of G. diazotrophicus (ATCC 49037) and the native isolation (GIBI029), and the subplot was divided into N and P fertilization levels. Five milliliters of each bacterial suspension (ATCC 49037 or GIBI029; 18 × 107 CFU/mL) were diluted to 1 L with distilled water and applied as a 75 mL soil drench per plant 20 days after transplanting (single application) [15]. For comparison, an absolute control or treatment without bacterial application was tested as well. In addition, canonical correlation analysis was performed to evaluate the relationships among soil and foliar variables. This analysis allowed the identification of associations between nutrient variables and provided a more integrated interpretation of soil–plant interactions under the evaluated treatments. The results were complemented with correlation matrices to facilitate the interpretation of interactions among variables. Furthermore, response surface analysis was applied to explore the interaction effects between N and P fertilization levels and their relationship with yield and selected soil and foliar variables. This approach allowed the visualization of response patterns and facilitated the interpretation of combined factor effects under the experimental conditions.
Different treatment combinations, including the addition or omission of bacterial suspensions and the application of either 100% of the soil’s required N or P chemical fertilizers, were evaluated. Treatments involving 100% N fertilization were performed by adding urea (BASF Co., Ltd., Limburgerhof, Germany) at a rate of 729 kg/ha. Treatments with 100% P fertilization were carried out by the addition of triple superphosphate (Crown Champion Industrial Co., Ltd., Tianjin, China) at a rate of 771 kg/ha. These rates were calculated from the soil analysis performed. The treatments of the experimental setup are presented in Table 1.

2.4. Soil Sampling and Analysis

Before crop sowing, 15–20 subsamples per hectare were collected at a depth of 20–40 cm following the methodology proposed by Kimel de Colombia [30], tracing imaginary zig-zag lines within the plot and taking random subsamples with an auger, avoiding the incorporation of vegetation cover. The collected soil was homogenized to obtain a 1 kg analytical sample in pre-labeled plastic bags.
Physicochemical soil characterization included the determination of texture using the Bouyoucos hydrometer technique and pH with a potentiometer and a soil:water suspension (1:2) [31]. Organic matter (OM) content was determined by wet oxidation and colorimetric quantification [32,33], total N by the Kjeldahl method [34], and available P by Bray II extraction and colorimetric quantification [35,36].
Exchangeable cations, including calcium (Ca), magnesium (Mg), sodium (Na), and potassium (K), were determined by ammonium acetate (1 M, pH 7) extraction followed by atomic absorption [37,38]. Microelements, including iron (Fe), copper (Cu), manganese (Mn), and zinc (Zn), were determined by EDTA extraction and atomic absorption [39,40]; sulfur (S) by monocalcium phosphate turbidimetric extraction [41]; and boron (B) by calcium monobasic phosphate Azometine-H colorimetric extraction [42,43].

2.5. Soil Preparation, Transplanting, and Crop Management

Soil was prepared by plowing to a depth of 25 cm and creating 20 cm wide furrows using a reinforced hoe. Subsequently, dolomitic agricultural lime was applied at 240 g per linear meter (equivalent to 1050 kg/ha), and organic fertilizer was incorporated at 360 g per linear meter (equivalent to 3000 kg/ha). The dolomitic agricultural lime (Cales Río Claro Ltda., Puerto Triunfo, Colombia) contained 55.93% CaCO3 and 42.95% MgCO3, corresponding to approximately 236 kg Ca/ha and 128 kg Mg/ha. The organic amendment consisted of Abonissa organic fertilizer (Incubadora Santander, Caloto, Colombia); according to the manufacturer, the product contains 15 g N/kg, 34 g available P/kg, and 35 g water-soluble K/kg. Based on the application rate used in this study (3000 kg ha−1), the amendment supplied approximately 45 kg N/ha, 102 kg available P/ha, and 105 kg water-soluble K/ha.
The soil was leveled with a rake and covered with a 1.2-gauge black plastic mulch for weed control. A drip irrigation system with emitters spaced 20 cm apart was installed to ensure the daily water requirements of the crop at different developmental stages. The irrigation time was adjusted according to the physiological phase.
Thirty days after sowing, when seedlings reached the three- to four-true-leaf stage, they were transplanted from the seedbed into the greenhouse. Plants were established at a spacing of 40 cm between plants and 120 cm between rows in a grid of 1.2 m by 0.4 m, resulting in a planting density of 20,833 plants/ha. The crop was fertilized based on soil analysis and according to the evaluated treatments, with additional nutrient sources supplied as required by the crop: MgSO4 (IFFCO Kisan Suvidha Ltd., New Delhi, India) at a rate of 520 kg/ha, which, according to the manufacturer, contained 99 g Mg/kg and 120 g S/kg, corresponding to 51.5 kg Mg/ha and 62.4 kg S/ha; KCl (Lvfeng Fertilizer Co., Ltd., Zibo, China) at 937 kg/ha, which, according to the manufacturer, contained 498 g K/kg, corresponding to 466.6 kg K/ha; and micronutrients (Yara International ASA, Oslo, Norway) at a rate of 205 kg/ha. Potassium chloride was selected because it is the standard potassium fertilizer used in local tomato production systems and was recommended based on the soil analysis and crop nutrient requirements; furthermore, the experimental soil did not show sulfur deficiency, making the use of potassium sulfate unnecessary as a sulfur source.
A split fertilizer application strategy was adopted from transplanting until 150 days after transplanting. N and P fertilizers were applied at transplanting and again at 30 and 60 days after transplanting, whereas KCl, MgSO4, and micronutrients were supplied at transplanting and at 30-day intervals until 150 days after transplanting according to crop nutritional requirements.
The crop was trained to a two-stem plant architecture. Subsequently, technical pruning, as described by Jaramillo et al. [28], was performed until the main stem reached 12 floral clusters. At this point, the apical bud was pruned to terminate plant growth. General crop management followed the protocols outlined by Jaramillo et al. [28] for tomato cultivation under semi-controlled conditions.

2.6. Foliar Tissue Characterization

At the end of the cultivation cycle (180 days after transplanting), 12 soil subsamples were collected at a depth of 20–40 cm, considering the treatment distribution map and the sampling procedure proposed by Kimel de Colombia [30]. Three subsamples were collected per block, and physicochemical soil characteristics were determined using the same variables evaluated in the initial soil analysis.
Sixteen days before the end of the cultivation cycle, three foliar tissue samples were collected in the field for each treatment, according to the experimental design. Foliar samples were taken from the same spot where soil samples were extracted, collecting from the middle and upper part of the plant, specifically the third or fourth fully expanded compound leaf from the base of the plant at the leaf-stem junction. A total of 20 to 30 leaves were collected per plant. Samples were placed in perforated plastic bags, labeled, and transported to the Universidad de Caldas’ Animal and Plant Nutrition Laboratory in a portable refrigerator with ice packs to maintain their integrity. Foliar samples were analyzed for moisture content, dry matter, and total N using the Kjeldahl method, P content by colorimetry, and potassium content by atomic absorption spectrophotometry.

2.7. Economic Analysis

To assess the economic feasibility of greenhouse tomato production, production costs for each treatment were determined based on the cost format outlined by the Agricultural Sector Price and Supply Information System (SIPSA) of the National Administrative Department of Statistics of Colombia (DANE) [44]. All monetary values are expressed in US dollars (USD). Tomato prices were estimated based on the average wholesale market value over the past five years (2019–2024) as reported by Corporación de Abastos de Bogotá S.A. [45], and weekly reports from DANE [44]. The yield values used for the economic analysis correspond to previously published data obtained from the same greenhouse experiment, using the same experimental design, treatments, crop management practices, and environmental conditions [15]. In the present study, these yield data were incorporated exclusively as input variables for the economic evaluation, whereas the soil and foliar chemical data constitute the novel experimental results reported herein.
The cost of the G. diazotrophicus suspension was estimated according to [46]. The techno-economic parameters used and the calculations performed to assess the economic viability of the tomato production system were described elsewhere [14]. Economic indicators, including unit production margin (UPM), benefit–cost ratio (B/C), gross income, net income, and direct and indirect production costs, were calculated for each treatment.

2.8. Statistical Analysis

To evaluate the impact of experimental factors and their interactions, data were subjected to an Analysis of Variance (ANOVA) using the General Linear Model (GLM) using SAS software (version 9.4; SAS Institute, Cary, NC, USA). Significant treatment effects were further analyzed through Duncan’s multiple-range test. All statistical evaluations were conducted at a significance threshold of p < 0.05.

3. Results

3.1. Soil Chemical Properties

Initial analysis of the Andisol soil showed an acidic pH of 4.8, together with low exchangeable concentrations of Ca (2.38 cmol/kg), Mg (0.65 cmol/kg), and K (0.19 cmol/kg). These conditions may limit tomato production, particularly under greenhouse cultivation. Although total P (144 mg/kg) and S (25.54 mg/kg) were classified as high and optimal (see Table S1 in Supplementary Material), their estimated plant-available concentrations drop to 14.4 and 15.32 mg/kg, respectively. This difference is relevant because acidic volcanic soils can strongly retain P by forming complexes with iron and aluminum [47]. In contrast, the concentrations of Fe, Mn, Zn, Cu, and B were classified as high or optimal. These results indicate that the initial soil condition was mainly constrained by acidity, low base saturation, and limited effective P availability, rather than by micronutrient deficiency (Table S1 in Supplementary Material).

3.2. Exchangeable Relationships Among Macronutrients

The exchangeable cation relationships, including (Ca2+ + Mg2+)/K+, Ca2+/Mg2+, Ca2+/K+, Mg2+/K+, K+/NO3, Ca2+/B3+, Fe/Mn, and P/Zn, provided additional information on the nutritional balance of the initial soil [48]. The sum of bases was 3.65 cmol/kg, which was within the lower limit of the reference range of 3–10 cmol/kg [49] (see Table S2 in Supplementary Material). While Ca remains the dominant soil cation, the Ca2+/K+ (<15) and Ca2+/B3+ (<1000) ratios confirm a clear Ca deficiency. In contrast, the Ca2+/Mg2+ ratio (3.66) was optimal. Both the (Ca2++Mg2+)/K+ (15.95) and Mg2+/K+ (3.42) ratios fell below minimum thresholds, directly limiting Ca and Mg availability. Additionally, Fe/Mn (>10) and P/Zn (<8) ratios favored the selective retention of Mn and Zn, while the deficient K+/NO3 ratio (0.36) threatens fruit quality, potentially causing soft texture and blotchy ripening [49].

3.3. Effect of the Addition of Fertilizers and G. diazotrophicus on the Soil

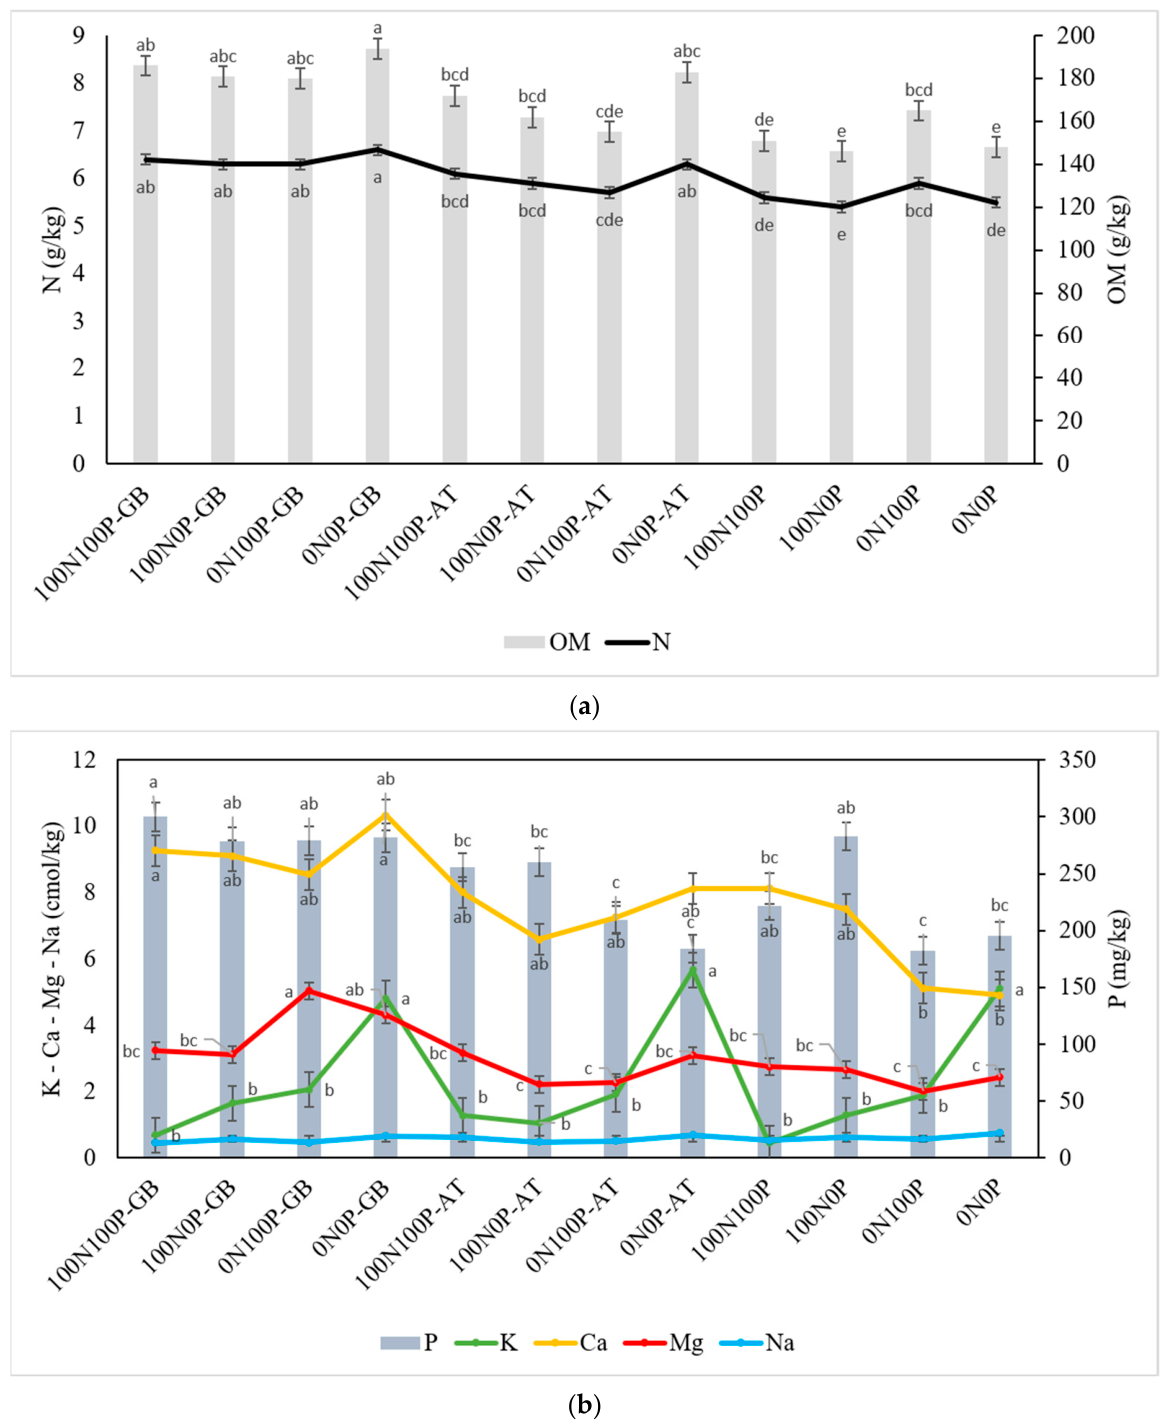
Figure 2 presents the impact of N and P fertilization levels on the nutrient content of a soil cultivated with tomato throughout its production cycle. Soil organic matter and edaphic N concentrations varied significantly across treatments (p < 0.05), demonstrating a strong positive correlation. The 0N0P-GB treatment showed the highest values, and treatments inoculated with the native GIBI029 isolate generally maintained higher organic matter and N concentrations than the reference strain and the non-inoculated controls (Figure 2a). In contrast, treatments inoculated with the ATCC 49037 reference strain showed lower organic matter and N values, particularly in the 0N100P-AT treatment. The non-inoculated controls also showed comparatively low values, with 100N0P presenting the lowest N concentration. These results indicate that GIBI029 inoculation was associated with greater residual soil organic matter and N after the crop cycle. However, these results should be interpreted as treatment-level differences and not as direct evidence of a specific microbial mechanism.
Figure 2b shows the response of soil P, K, Ca, Mg, and Na. Treatments inoculated with GIBI029 were associated with higher available P and exchangeable base concentrations than the corresponding ATCC 49037 and non-inoculated treatments. Treatments inoculated with either bacterial type also tended to maintain higher Ca2+ and Mg2+ concentrations than the non-inoculated controls. However, because no significant interaction between bacterial inoculation and fertilization was detected, these differences should be interpreted as treatment-specific responses rather than evidence of interaction effects. Soil K showed a different pattern from the other nutrients. The highest K accumulation was observed in the 0N0P treatment, which may reflect reduced plant uptake under conditions of primary macronutrient limitation. Na remained low across all treatments and was not markedly affected by the inoculation or fertilization treatments. Overall, these observations describe differences among treatments and should not be interpreted as evidence of a significant interaction between inoculation and fertilization.
The ANOVA indicated that the bacterial application significantly altered several soil chemical properties. The treatment factor exerted a highly significant effect (p < 0.01) on soil organic matter (p = 0.0085), N (p = 0.0045), and K (p = 0.0001), highlighting high sensitivity in K dynamics. Significant effects (p < 0.05) were observed for P (p = 0.0423), Ca (p = 0.0216), and Mg (p = 0.0123). On the other hand, Na concentrations remained statistically unaffected by the treatments (p = 0.6354), maintaining a uniform mean of 0.58 cmol/kg. The block effect showed no significant influence (p < 0.05) on any edaphic variable, indicating adequate spatial homogeneity of the experimental design and confirming that variations resulted exclusively from the evaluated applications (Table S3 in Supplementary Material).
In general, most treatments exhibited a cationic imbalance between Ca, Mg, and K (see Table 2). Among the twelve treatments evaluated, only 100N100P and 100N100P-GB showed optimal or near-optimal Ca2+/K+ ratios, with values of 18.2 and 13.2, respectively (see Table S1 in Supplementary Material for reference values). These same treatments also showed suitable (Ca2+ + Mg2+)/K+ ratios according to the reference range of 20–40 cmol/kg proposed by Sánchez [49].
Optimal K+/NO3 ratios were observed in 100N100P-GB and 100N0P-AT (Table 2). Most remaining treatments showed ratios above 2, which has been associated with green shoulder development in tomato fruits. The 100N100P treatment, without bacterial inoculation, showed a K+/NO3 ratio below 1, which has been linked to soft or blotchy fruits [49]. In addition, Mg2+/K+ ratios were below the optimal range of 4–6 in ten of the twelve treatments, indicating a possible Mg imbalance. The sum of exchangeable bases (Ca2 + Mg2 + K+ + Na+) was highest in the 0N0P-GB treatment and moderate in the remaining treatments.

3.4. Foliar Tissue Analysis and Yield Performance

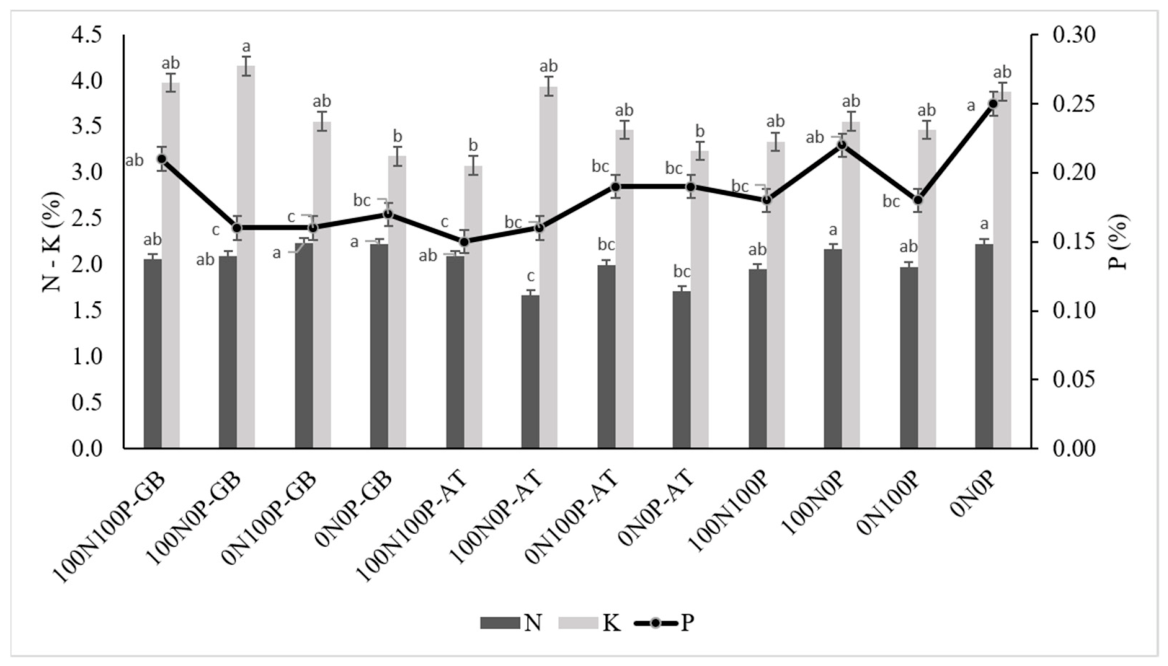
Foliar tissue analysis showed significant differences in N content among treatments (p < 0.05) (Figure 3). The lowest foliar N concentrations were observed in 0N0P-AT and 100N0P-AT, with values of 17.1 and 16.7 g/kg, respectively. In contrast, treatments inoculated with the native GIBI029 isolate generally showed higher foliar N concentrations.
The yield data presented in Table 2 were previously reported by Ceballos-Aguirre et al. [15] from the same greenhouse experiment and under identical treatment conditions. These values are included here solely to establish the relationship between soil and foliar nutrient responses and the corresponding economic performance of each treatment. Therefore, the novelty of the present study lies in the integrated analysis of soil chemical properties, foliar nutrient composition, and economic outcomes.
Figure 3 and Table 2 show that the highest foliar K concentration was observed in 100N0P-GB, with 41.6 g/kg. This treatment also showed a high yield of 98.0 t/ha. Because no significant interaction between fertilization and bacterial type was detected, these comparisons are presented only to describe the observed treatment responses. Treatments inoculated with GIBI029 generally showed high foliar K concentrations. However, the 0N0P-GB treatment showed a lower foliar K concentration of 31.8 g/kg while still reaching one of the highest yields, 106.1 t/ha. In contrast, 100N0P-AT showed a foliar K concentration of 39.4 g/kg, but its yield was less than half of that obtained with 100N0P-GB. The non-inoculated treatment receiving both N and P showed a foliar K concentration below the treatment average of 35.7 g/kg.
Among the evaluated treatment combinations, 100N0P-GB and 100N100P-GB showed similar foliar K concentrations of 41.6 and 39.8 g/kg, respectively. Their corresponding yields were also high, reaching 98.0 and 106.4 t/ha, respectively (Figure 3 and Table 2). These comparisons are descriptive and should not be interpreted as evidence of a significant interaction between fertilization and bacterial type.
Regarding P foliar content, the treatment without the addition of N and P (0N0P) exhibited the highest P concentration among all treatments (2.5 g/kg). In contrast, the treatment with full N and P fertilization in the presence of the ATCC 49037 strain (100N100P-AT) displayed the lowest P content (Figure 3).
In general, the analysis of variance (Table S4 in Supplementary Material) indicated that both bacterial type and fertilization treatments influenced foliar nutrient composition, with significant differences (p < 0.05) observed primarily for N, P, and K contents. Among these variables, N content showed the most consistent differentiation across treatments, particularly in response to bacterial inoculation. No significant interaction was detected between fertilization levels and bacterial type for the evaluated foliar variables.

3.5. Canonical Correlation Analysis Applied to Foliar and Soil Variables

Table 3 presents the correlation matrix among foliar variables. This matrix revealed generally weak to moderate possible relationships among the evaluated foliar variables, with only a few statistically meaningful associations. A significant positive correlation was observed between potassium and phosphorus (r = 0.54), indicating a potential synergistic interaction between these nutrients, likely associated with their complementary roles in plant metabolic and energy-transfer processes. In contrast, nitrogen exhibited a moderate negative correlation with potassium (r = −0.30), suggesting possible antagonistic uptake dynamics under the studied conditions.
Moisture and dry matter displayed a perfect negative correlation (r = −1), reflecting their intrinsic inverse relationship as complementary physiological components. P showed weak to moderate possible associations with other variables, including a negative relationship with nitrogen (r = −0.26) and moisture (r = −0.21), and a positive relationship with dry matter (r = 0.21), indicating subtle variations in nutrient allocation and tissue composition. Additionally, ash content exhibited a strong positive correlation with K (r = 0.77) and a moderate relationship with P (r = 0.47), suggesting that mineral accumulation in plant tissues is largely driven by these elements.
The correlation analysis of soil variables (Table 4) revealed several relevant associations, indicating patterns of co-variation among key edaphic properties. A very strong and significant positive correlation was observed between organic matter (OM) and nitrogen (r = 0.99), indicating their possible close interdependence and highlighting the possible role of organic matter as a primary reservoir and regulator of nitrogen availability in soil systems. This result is consistent with the well-established relationship between soil organic matter and nitrogen availability reported in previous studies [50,51]. Moderate positive correlations were found between organic matter and the exchangeable Ca2+ (r = 0.33) and Mg2+ (r = 0.42), as well as between N and these same cations (Ca2+: r = 0.33; Mg2+: r = 0.43). These results suggest that soils with higher organic content may tend to promote greater retention of base cations. Available P showed moderate positive associations with Ca2+ (r = 0.40) and Mg2+ (r = 0.49), and a negative association with K+ (r = −0.28). These patterns may reflect contrasting nutrient dynamics in Andisols, where P behavior is strongly influenced by mineral components and fixation processes [52,53]. K+, in turn, showed a moderate positive correlation with Na+ (r = 0.51), suggesting similarities in exchange behavior within the soil matrix. A significant positive correlation between calcium and magnesium (r = 0.59) was also observed, consistent with their co-occurrence in soil exchange complexes.
A trend was observed in soil nutrient dynamics determined by the interrelated relationships among organic matter, macronutrients, and exchangeable cations. Overall, the correlation analysis showed that soil and foliar nutrient responses were complex and not always directly coupled. Most correlations were weak or moderate, indicating that plant nutrient composition was influenced by several interacting physiological and environmental factors rather than by simple linear relationships.
Despite this, soil P and K levels showed relatively weak associations with their corresponding foliar concentrations [52,54]. This pattern suggests that soil nutrient concentrations alone may not fully explain nutrient accumulation in plant tissues. However, because correlation analyses do not establish causal relationships, these results should be interpreted as associations rather than evidence of specific soil–plant nutrient mechanisms. For example, P availability is known to depend on its chemical form and degree of fixation in the soil, particularly in Andisols, where different P pools may vary considerably in their bioavailability to plants.
To facilitate the interpretation of the complex interactions among soil and foliar variables, a correlation heatmap was constructed. This graphical representation integrates the relationships depicted in Figure 4, allowing for a more comprehensive visualization of both positive and negative associations within the soil–plant system.
The heatmap clearly highlights the strong coupling between soil organic matter and total N, as well as the antagonistic interactions involving K, P, and Mg at the foliar level. In contrast, soil P and K showed weaker relationships with their foliar concentrations, suggesting partial decoupling between nutrient availability and plant uptake. This indicates that nutrient assimilation is not only related to the total concentration in soil, but also to physicochemical conditions and biological interactions in the rhizosphere [52]. In addition, the heatmap shows antagonistic interactions among some nutrients, especially between Mg and K, and also between high N conditions and foliar P levels, reflecting possible competition during uptake and some ionic imbalance in the plant. In general, these results suggest that nutrients are interacting in a coordinated way rather than independently. This behavior can help explain the differences observed in yield, indicating that productivity is more related to nutrient balance than to the increase of a single element.

3.6. Response Surface Analysis of Macronutrients and Yield at the Soil and Foliar Levels

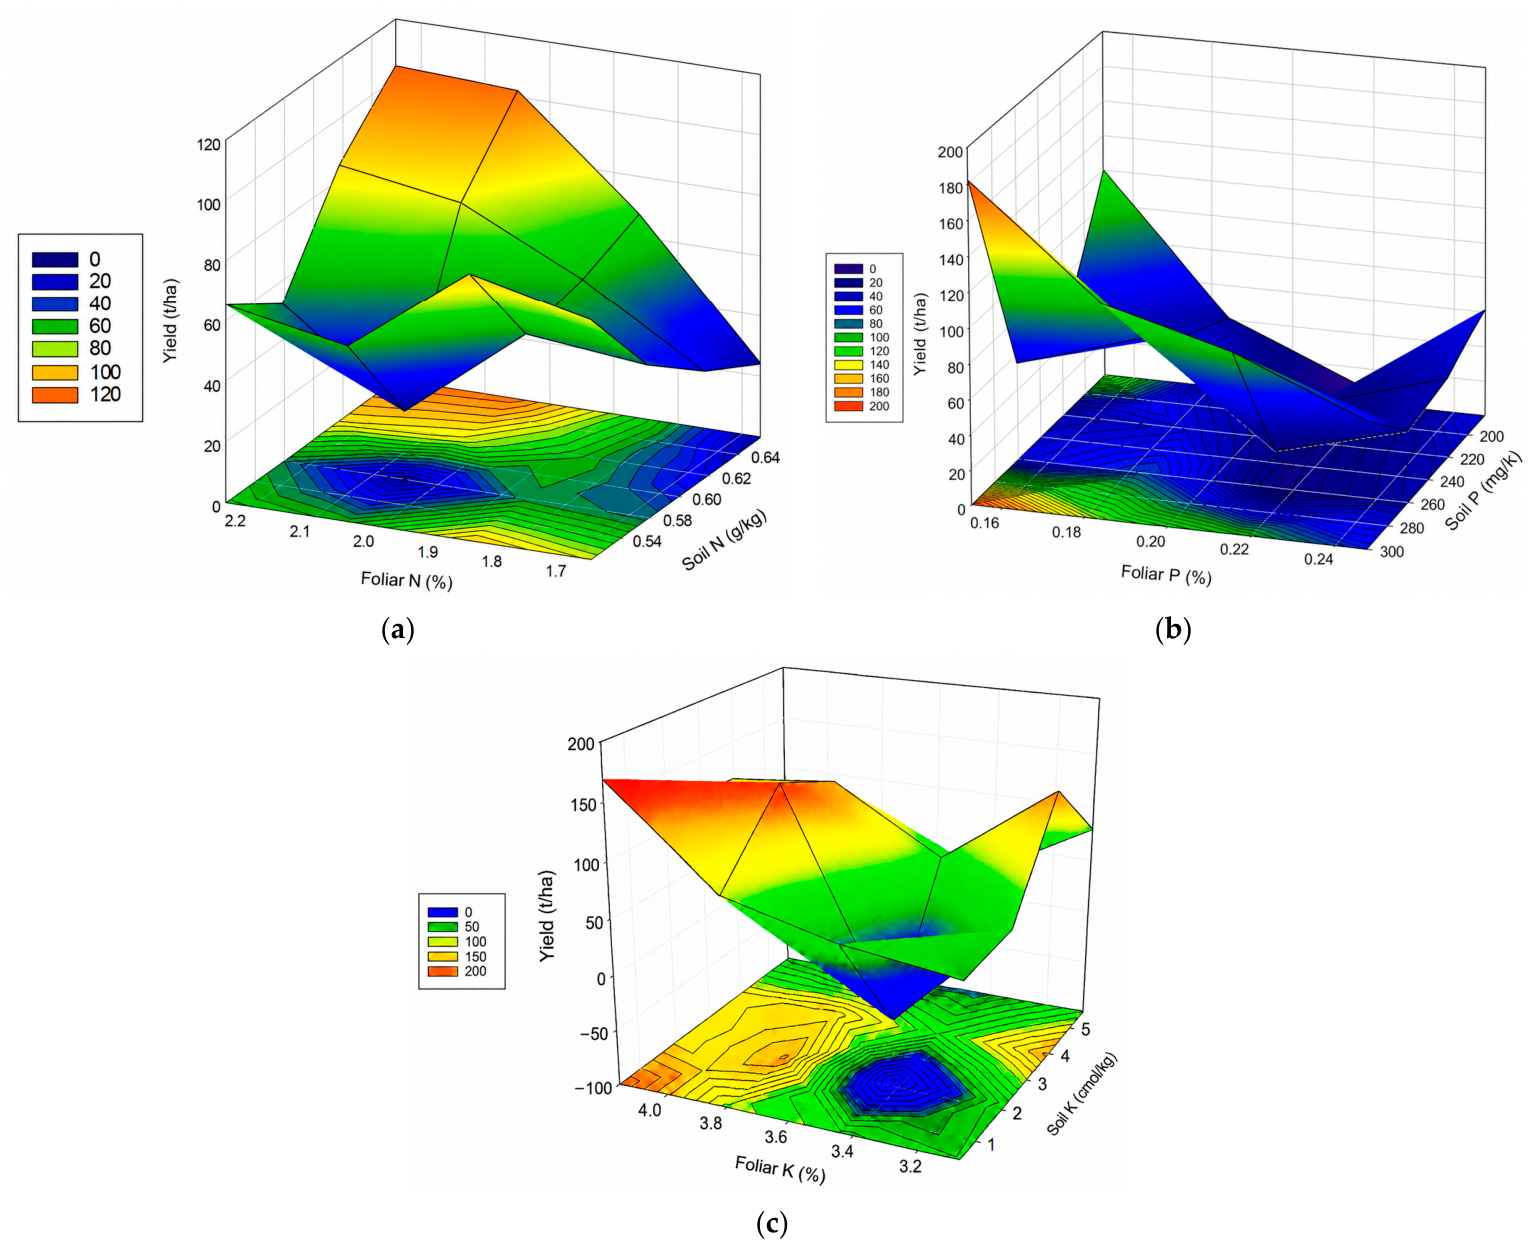
The response surface model derived from the analysis of N, P, and K clearly indicates that crop yield is governed by a complex and non-linear interaction among these elements, rather than by the isolated effect of any single nutrient (Figure 5). Overall, the model reveals that productivity is highly dependent on nutrient balance, with optimal yields occurring within specific intermediate combinations of these macronutrients at both soil and foliar levels.
It is worth highlighting the N contents, particularly within the ranges of 0.56–0.64% in soil and 1.67–2.23% in plant tissue, where higher yields were associated with treatments inoculated with the GIBI029 isolate and supplemented with fertilization (Table 1).
The N–P surface showed a clear response pattern in which maximum yield occurred at intermediate levels of both nutrients. The highest concentrations of N and P did not correspond to the highest yield values. This result supports the importance of balanced nutrient supply in greenhouse tomato production.
The N–K and P–K surfaces also showed non-linear yield patterns across the evaluated nutrient ranges (Figure 5). In both cases, higher yield values tended to occur at particular combinations of nutrient levels.
The response surface showed non-linear response patterns across the evaluated nutrient combinations. These graphical surfaces illustrate overall treatment trends and are intended to facilitate the visualization of the observed responses. Because no significant interaction effects were detected in the ANOVA, and no formal interaction tests were performed within the response surface analysis, these patterns should be interpreted as descriptive associations rather than evidence of statistically significant nutrient interactions or causal relationships.

3.7. Economic Assessment

The economic analysis presented in this study is based on previously validated yield data [15], which are integrated with newly obtained soil and foliar chemical information (see Table 5). This analysis of the treatments reveals substantial differences in profitability associated with fertilization and inoculation strategies. Treatments involving inoculation with the native G. diazotrophicus isolate yielded the highest gross revenues (≥28,800 USD/ha) and positive net profits, with the 0N0P-GB treatment standing out in particular, as it achieved the highest net income (20,106 USD/ha) and the best benefit-to-cost ratio (B/C = 2.65), indicating high economic efficiency even in the absence of chemical fertilization. Similarly, the 100N100P-GB and 100N0P-GB treatments showed high net profits (18,259 and 16,482 USD/ha, respectively) and B/C ratios greater than 2.2, suggesting that inoculation significantly improves economic returns regardless of the fertilization level. In contrast, treatments with the inoculation of the ATCC reference strain had considerably lower gross revenues (≈11,348–14,420 USD/ha) and, in several cases, negative profitability (e.g., 0N0P-AT at −825 USD/ha), reflecting low productive and economic efficiency. Treatments without inoculation showed intermediate results, with moderate profits (1321–5320 USD/ha) and B/C ratios between 1.1 and 1.45, indicating limited profitability compared to treatments with the application of the native isolate GIBI029 (Table 5).
In terms of yield and economic efficiency (UPM), treatments with the application of the GIBI029 isolate had lower unit production costs (0.11–0.14 USD/kg), while the treatments with the application of the ATCC reference strain showed the highest values (0.27–0.33 USD/kg), indicating lower production efficiency. Overall, the results indicate that inoculation with G. diazotrophicus may not only increase crop yield but also has the opportunity to optimize the profitability of the production system (see Table S5 in Supplementary Material), emerging as an economically viable and sustainable alternative to conventional fertilization strategies.

4. Discussion

The changes observed in soil chemical properties indicate that nutrient dynamics in greenhouse tomato production were influenced by both fertilization strategy and microbial inoculation. Across the measured variables, the native isolate GIBI029 was more consistently associated with a favorable residual soil chemical profile, higher foliar N, higher previously reported yield, and better economic indicators than the reference strain ATCC 49037 and the non-inoculated controls. At the same time, the multivariate analyses support associative rather than mechanistic interpretations. Likewise, the economic assessment should be interpreted as scenario-based because it used previously published yield data from the same experiment, and no formal statistical comparison of economic indicators was performed.

4.1. Baseline Soil Constraints and Residual Cation Balance

The soil was strongly acidic (pH ≈ 4.8), which is below the optimal range for the availability of several crop nutrients. In such acidic Andisols, P often becomes fixed (forming insoluble complexes), whereas micronutrients such as Fe, Mn, Zn, and B tend to be more soluble. The initial pH, together with low exchangeable Ca, Mg, and K, indicates a system in which nutrient imbalance was already likely before transplanting. This condition is especially relevant in Andisols because extractable P may appear high, even when its effective availability to plants remains restricted by strong retention in the soil matrix. Under these soil conditions, crop performance is more likely to depend on the combined regulation of pH-sensitive nutrient availability, cation balance, and root-zone processes than on the concentration of a single element [55,56,57].
The post-harvest cationic relationships confirm that this nutritional context remained important throughout the crop cycle. Only a few treatments approached suitable Ca2+/K+ and (Ca2+ + Mg2+)/K+ ratios. In contrast, most treatments still showed low Mg2+/K+ or Ca2+/K+ values, which point to persistent imbalance in the exchange complex. This is agronomically relevant because tomato productivity is highly sensitive to the balance among base cations, not only to their isolated concentrations [58]. At the same time, the treatment inoculated with GIBI029 and without external N or P fertilization (0N0P-GB) showed the highest sum of exchangeable bases. This suggests a more favorable residual fertility status than that observed in the corresponding non-inoculated treatment and in the treatments inoculated with ATCC 49037. These patterns indicate that the native isolate improved the chemical profile of the production system. However, they also show that biofertilization did not fully overcome the structural nutrient constraints associated with the acidic soil [55,59,60].

4.2. Soil Chemical Response to Inoculation and Fertilization

The clearest soil response in this study was the contrast between bacterial treatments. Across fertilization regimes, the native isolate GIBI029 was associated with higher organic matter, total N, available P, exchangeable Ca, and exchangeable Mg. The values associated with this isolate reached 185.1 g/kg organic matter, 6.4 g/kg total N, 284.75 mg/kg available P, 9.32 cmol/kg exchangeable Ca, and 3.93 cmol/kg exchangeable Mg. In contrast, fertilization level alone affected a narrower group of variables and showed a clear statistical effect mainly on K. Because the fertilization × bacterial type interaction was not significant in the ANOVA, this pattern should be interpreted mainly as an effect associated with strain identity. It should not be taken as evidence that the isolate behaved differently under each fertilization combination in a statistically distinct way.
K followed a different pattern from the other soil variables. Residual soil K was highest in the unfertilized treatments and decreased when N and/or P were supplied. This behavior is more consistent with stronger crop demand and removal under more nutritionally active plants than with a direct depletion effect caused by inoculation itself. Likewise, soil P was higher in treatments that received N, with the maximum value observed in 100N0P treatment. In an Andisol, these patterns probably reflect the joint effect of fertilizer input, plant uptake, and P retention in the soil matrix. Therefore, the superior performance of GIBI029 is consistent with more favorable rhizosphere nutrient turnover and mobilization. Although the present data do not demonstrate biological N fixation, P solubilization, or any other specific mechanism directly in the plant, they can indicate the possible incidence of the growth-promoting properties caused by the bacterial inoculant [13,55,61]. In this sense, the agronomic response observed here strongly suggests that the native isolate modified nutrient dynamics in a favorable way, but the present dataset supports this conclusion at the level of soil and plant performance, not at the level of biochemical proof. This more cautious interpretation is also more consistent with the strain-specific nature of plant growth-promoting responses reported for G. diazotrophicus and other PGPR [13,56].
Some studies have reported that N can enhance P availability by altering soil pH through acidification or by modifying microbial activity. For instance, plant roots excrete organic acids that can solubilize insoluble P compounds, especially when N is applied [62]. Similarly, the combined application of N and P, as in the 100N100P treatment, maximizes plant growth, which in turn increases P uptake compared to conditions of deficiency. Jiang et al. [63] observed that agroecosystems with P-deficient soils exhibited a greater response to combined N and P inputs compared to those where P was more readily available. These findings underscore the importance of tailoring fertilization strategies to the specific characteristics of each soil and crop type. Imbalanced fertilization, such as the sole application of N without P, can lead to nutrient imbalances that may impair plant growth and negatively impact crop yield.
Jaramillo et al. [28] state that tomato vegetative development occurs best in soils with high organic matter content (above 5%), adequate nutrient supply, and pH values between 5.8 and 6.8. These conditions are also compatible with the growth requirements of G. diazotrophicus. Therefore, the response observed in this study may be related to the adaptation of the bacterial isolate to the edaphoclimatic conditions of the study area.
Salinity was unaffected by the bacterial strain, as the highest Na levels were observed in the absence of bacteria. This outcome aligns with G. diazotrophicus’ known growth characteristics, including an optimal temperature of 30 °C and a pH tolerance ranging from 2.5 to 6.0 [13].

4.3. Foliar Tissue Analysis and Yield Performance

When the foliar data are interpreted together with the previously published yield data from the same experiment, N becomes the clearest nutritional discriminator among treatments. The lowest foliar N values were observed in 0N0P-AT and 100N0P-AT (1.71% and 1.67%, respectively), whereas treatments inoculated with GIBI029 reached up to 2.24% foliar N and consistently maintained N near or above the treatment average. This pattern was agronomically relevant because the lowest foliar N values were associated with the lowest yields. By comparison, GIBI029 treatments produced between 94.7 and 106.4 t/ha under contrasting fertilization regimes [15].
K and P showed a less direct relationship with productivity. The highest foliar K values were recorded in 100N0P-GB and 100N100P-GB, with 41.6 and 39.8 g/kg, respectively, and both treatments were highly productive. However, 0N0P-GB treatment also corresponded to one of the highest yields (106.1 t/ha) despite having a lower foliar K concentration (31.8 g/kg). Likewise, the highest foliar P concentration was found in the uninoculated 0N0P treatment, with 2.5 g/kg, but this did not correspond to the highest yield. In this sense, these results suggest that tomato productivity in this system depended more on coordinated nutrient status than on the maximum accumulation of a single nutrient. This interpretation is consistent with the importance of nutrient balance in protected tomato production and with the known effect of K–N and Ca–K relationships on fruit development and physiological stability [19,50,58].
Although some K values were below the study average of 35.7 g/kg, foliar K uptake was still sufficient to support yields close to 106 t/ha when balanced with other nutrients. This indicates that increasing K concentration alone is not necessarily required to enhance yield. Physiologically, this could be explained by a luxury consumption response, where the plant has an abundant supply of an element and continues to take it up at the expense of yield [64]. The 100N0P-AT treatment can exemplify this phenomenon: it exhibits high K levels but ranked fourth-lowest in yield among all treatments assessed.
The integration of foliar nutrient status with the previously published yield dataset also strengthens the agronomic interpretation of the native isolate. The yield data were not generated again in the present study, but their use is justified because they belong to the same greenhouse experiment, under the same design, treatment structure, crop management, and environmental conditions [15]. In this context, the combined foliar and yield results indicate that the better performance associated with GIBI029 may be linked to a more favorable plant nutritional status, especially for N. This response should not be interpreted as a simple increase in tissue concentrations of all nutrients.

4.4. Canonical Correlation Analysis Applied to Foliar and Soil Variables

The correlation analysis was useful as an integrative tool, but it should be interpreted as evidence of association rather than causation. The strongest soil relationship was the near-perfect coupling between organic matter and total N (r = 0.99), which is expected because soil organic matter is a major N reservoir. Ca and Mg were also positively associated (r = 0.59), indicating their coupled behavior in the exchange complex. At the foliar level, P and K were positively correlated (r = 0.54), whereas moisture and dry matter showed the expected inverse relationship. These patterns are useful because they indicate how the soil–plant system responded as a whole, particularly the treatments that included microbial inoculation [56,57].
On the other hand, the soil–plant matrix suggested that higher soil organic matter and N tended to coincide with lower foliar K and P. This pattern may reflect nutritional competition, dilution effects, or shifts in root uptake selectivity, but the correlation analysis cannot identify which process predominated. The same applies to the weaker links between soil P or K and their foliar expression. In practical terms, the correlation structure supports the view that nutrient acquisition in this experiment was regulated by whole-system balance rather than by the abundance of isolated nutrients in the soil [58]. For this reason, the canonical correlations are better interpreted as an explanatory framework for integrated treatment responses than as evidence of direct mechanistic pathways.

4.5. Nutrient Interaction Patterns Suggested by the Response Surfaces

The high N levels in the 0N0P-GB treatment, together with yields exceeding 100 t/ha, indicate that yield response was not strictly proportional to N accumulation. Instead, crop performance appears to have depended on nutrient balance and coordinated availability rather than on the isolated increase of individual elements.
The response surfaces reinforce this integrative interpretation. Maximum yields were not associated with the highest concentrations of all nutrients, but with intermediate combinations of N and P, and with specific K ranges. This result is agronomically coherent with the general concept of nutrient balance and with the idea that the crop response depends on coordinated supply rather than on maximum dose. In the present case, the curvature of the surfaces was visually steeper along the N axis than along the P or K axes, which suggests that yield was more sensitive to N variation within the explored domain. However, this should be read as a descriptive pattern of the fitted surfaces and not as a formal ranking of factor importance.
The same caution applies to the interpretation of interaction patterns. The surfaces for N × P and N × K clearly show combined response zones, but they should not be interpreted as proof that all pairwise interactions were statistically significant in the ANOVA. In this study, the most defensible conclusion is that high yield required balanced nutrient combinations and that the native isolate performed more consistently across those combinations. This is agronomically more relevant than suggesting that one nutrient alone controlled the system [59].
This integrated response also suggests a possible role of bacterial inoculation in improving nutrient dynamics. The results may suggest that inoculation supported more favorable P and K mobilization and availability, facilitating their interaction with N and contributing to more efficient nutrient use. However, these interpretations should remain cautious because direct mechanistic measurements were not performed. The effect of G. diazotrophicus on soil chemical properties and foliar macronutrient content is largely associated with the endophytic behavior of each strain, which is influenced by its adaptation to specific crops and edaphoclimatic conditions. This bacterium has been isolated from diverse agricultural ecosystems, including sorghum, pineapple, and rice [65], and has also been reported to occur naturally in crops propagated by seed with low levels of readily assimilable sugars, such as cereals and coffee (Coffea arabica L.), where it performs various endophytic functions.
These findings help explain the contrasting performance observed between the native GIBI029 isolate and the reference strain ATCC 49037 (PAL 5). Although both strains were originally isolated from sugarcane, their origin in different agroecological environments resulted in markedly different responses under the evaluated conditions, reflecting differences in their microbial physiology. In this study, GIBI029 indicated a superior adaptability, likely due to its native origin, which allowed it to adjust more efficiently to the environmental conditions of the study area. In contrast, the reference strain PAL 5, originating from a different ecosystem, may have experienced limitations associated with environmental adaptation and microbial competition. In agreement with these observations, Mamani-Rojas et al. [66] reported that microbial performance was primarily associated with the agroecological conditions of origin rather than with the host plant, highlighting the relevance of selecting indigenous strains adapted to local environments to obtain stable and efficient biological responses.

4.6. Economic Assessment

From a practical perspective, the economic analysis indicates that the agronomic advantages associated with the native isolate may also translate into improved production profitability under the evaluated greenhouse conditions. The economic results extend the agronomic interpretation, but they should be interpreted with methodological caution. The economic indicators were calculated from the yield data previously published for the same greenhouse experiment and were combined here with the new soil and foliar results in order to evaluate the production system as a whole [15]. Under the prices and costs used in this analysis, the GIBI029 treatments generated the most favorable indicators—especially 0N0P-GB, which combined the lowest unit production margin (0.11 USD/kg), the highest net income (20,106 USD/ha), and the highest benefit–cost ratio (2.65). The fully fertilized treatment with GIBI029 was also favorable (B/C = 2.29), whereas the ATCC treatments ranged from near equilibrium to negative returns.
These contrasts are agronomically meaningful because they show that the native isolate did not simply sustain yield; it can also improve the economic efficiency of the input structure. This result is particularly important for greenhouse tomato, where profitability depends strongly on fertilizer cost and marketable yield. Nevertheless, the economic assessment should be interpreted as a comparative scenario rather than as a statistical demonstration of commercial superiority, because the economic indicators were not subjected to inferential analysis and profitability will necessarily vary with tomato prices, labor costs, and inoculant cost. Within those limits, the results obtained here support the native isolate, particularly under low-input management, as the treatment option that generated the most favorable agronomic–economic balance in this study [14,15].
Unlike previous studies focused exclusively on yield response, this work integrates agronomic, physicochemical, and economic dimensions, providing a more holistic understanding of the role of G. diazotrophicus in sustainable tomato production systems.

4.7. Comparative Analysis with Previous Studies

The present results are consistent with the broader literature showing that microbial inoculants only improve crop nutrition when there is functional compatibility between strain, host plant, and management conditions [60,67]. For tomato, previous work with G. diazotrophicus has already shown positive responses in field production [11], seedling growth and P-dependent effects [12], in vitro plant growth-promoting traits in Colombian isolates [13], technical and economic benefits under protected conditions [14], and high yield of the same native isolate under contrasting N and P regimes [15]. The present study extends that line by integrating post-harvest soil chemistry, foliar composition, previously validated yield data, and economic performance within the same experimental framework. It also agrees with other tomato studies in which PGPR improved nutrient status, soil quality, or yield, although the magnitude of the response depended on the inoculant and the production context [16,17,18,19].
The interpretation is also consistent with results from other vegetables. Positive effects of PGPR on soil nutrient availability, leaf nutrient concentration, and crop productivity have been reported in pepper [20], lettuce [21], and pak choi [22], whereas cucumber responses vary strongly with nutrient supply and inoculation context [23]. A related positive interaction between G. diazotrophicus and N/P fertilization has also been reported for carrot in field conditions [29]. In this sense, these studies support the idea that the association observed here was not a generic “biofertilizer effect”, but a system-specific response linked to strain identity and nutritional context.
Studies in strawberry [9], maize [68], carrot [69], and sugarcane [70] point in the same general direction. In strawberry, G. diazotrophicus improved P and Fe nutrition under specific nutritional stress conditions [9,10]. In maize, carrot, and sugarcane, inoculation has been associated with improved soil fertility, stronger plant performance, and a partial reduction in the dependence on mineral fertilization, especially when combined with other beneficial microorganisms or adjusted nutrient management. At the same time, mechanistic and ecological studies show that strain performance depends on gene-level traits [7,8], colonization behavior [57,71,72], and the surrounding diazotrophic community [55,56,73,74]. For that reason, the present results should be interpreted as agronomic evidence of strain-specific performance by GIBI029, not as direct proof of the mechanism involved. The distinctive contribution of this study is therefore the integrated demonstration that a native isolate can improve residual soil fertility, foliar N status, yield, and economic outcome in greenhouse tomato within a single experimental framework.
Although the crop management practices adopted in this study were implemented in 2022 following the technical recommendations of Jaramillo et al. [28], recent studies indicate that these agronomic principles remain valid. Farneselli et al. [61] highlighted that efficient irrigation scheduling, balanced fertilization, and the integration of biological inputs remain key components of sustainable tomato production systems. This agreement between earlier technical recommendations and more recent evidence supports the relevance of the crop management strategy adopted in the present study.
Beyond the agronomic and economic outcomes observed in this study, the practical application of these findings has already progressed beyond the experimental stage. Previous research with the native GIBI029 isolate has allowed the optimization of inoculation dose, application timing, yield response, fruit quality attributes, and fertilizer management strategies. Based on these advances, the isolate has been incorporated into a stabilized microbial inoculant developed through collaboration between academic institutions and private-sector partners. This biofertilizer has been evaluated under commercial farming conditions in the study region and neighboring areas, where it has contributed to maintaining crop productivity while reducing dependence on synthetic fertilizers and supporting soil fertility management. Therefore, the results obtained in the present study not only provide new associations regarding soil and foliar nutrient dynamics but also strengthen the scientific basis for the future adoption of G. diazotrophicus-based biofertilizers as a sustainable tool for greenhouse tomato production and other horticultural systems under tropical conditions.

4.8. Limitations of This Study

This study has some limitations that should be considered when interpreting the effect of G. diazotrophicus on the soil’s chemical profile in greenhouse tomato. The experiment was conducted in a single greenhouse cycle and in one soil-climate context. The soil was an acidic Andisol showing particular P dynamics. Therefore, the responses observed here should be interpreted mainly for this crop–soil management combination. They should not yet be extrapolated to open-field systems or to soils with different baseline fertility. This is in agreement with previous reports showing that inoculation responses depend on nutrient availability, crop genotype, and growing environment [9,12,59,75].
This study also has inherent limitations because it did not incorporate new mechanistic measurements. In particular, endophytic colonization of G. diazotrophicus in tomato tissues was not quantified, nor was biological N fixation in planta directly measured (e.g., through isotopic tracers or molecular markers). Therefore, although the observed patterns in soil properties, foliar nutrition, yield, and profitability are consistent with a plant growth-promoting effect reported in the literature, the mechanistic inferences should be interpreted as plausible rather than conclusive. Nevertheless, the experimental design, including comparative treatments (native isolate vs. reference strain vs. control; N/P combinations; block replication), supports important conclusions regarding agronomic performance and economic feasibility under local conditions.
Only two bacterial strains were compared, and inoculation was evaluated under one application timing, one delivery strategy, and one dose. Therefore, the better performance of GIBI029 should be interpreted as a strong strain-specific result, but not as evidence that all G. diazotrophicus inoculants will behave similarly. Recent reviews indicate that strain identity, inoculation procedure, carrier quality, persistence, and formulation can strongly affect agronomic response [56,60]. In addition, although the design was adequate for major treatment contrasts, the level of replication may still limit statistical power for subtle interactions among strain, fertilization regime, and spatial soil variability.
Finally, the study relied mainly on soil and foliar end-point measurements and did not include direct mechanistic assays. Thus, the increases in N, P, or other nutrients cannot be attributed only to biological N fixation or solubilization, because in tomato and other systems, G. diazotrophicus effects are also related with the functionality of nif genes [7], colonization dynamics [57], and interactions with resident microbiota [5]. The economic assessment should also be interpreted as scenario-based, because profitability can change with local prices, labor, inoculant cost, and seasonal risk. Overall, these limitations do not invalidate the present results, but they indicate that the mechanistic interpretation and the wider agronomic applicability should still be made with caution.

4.9. Future Research

Future research should focus not only on improving the understanding of the mechanisms of G. diazotrophicus, but also on facilitating its application as a biofertilizer in horticultural systems. It is important to connect the agronomic results observed with the biological processes involved. For this purpose, future studies should include direct measurements such as endophytic colonization in plant tissues, biological N fixation using isotopic techniques (e.g., 15N), and evaluation of functional genes (e.g., nif genes). These analyses can be complemented with tools such as qPCR, microscopy, and omics approaches to better understand plant–microbe interactions. Another important aspect is to study the temporal dynamics of nutrient availability and plant uptake during the crop cycle. The present study shows final results, but future work should include sampling at different stages in order to identify when the inoculation has the greatest effect. This will help to optimize the timing of application.
From an agronomic point of view, it is necessary to validate the results obtained with the native isolate GIBI029 under different conditions. This includes trials in different soils, climates, and production systems (greenhouse and open field), as well as in other horticultural crops. These studies will help to confirm the consistency of the response and the range of application of the microorganism. It is also important to optimize the inoculation strategy, including dose, frequency, and method of application (such as seed coating, root inoculation, or fertigation). In addition, more work is needed on formulation, including carrier selection, shelf life, microbial viability, and compatibility with agricultural inputs. The use of microbial consortia could also be explored to improve the overall effect.
Future research should also include economic and environmental evaluations under commercial conditions. Long-term studies should assess reductions in chemical fertilizers, changes in soil health, and potential environmental benefits. Finally, these research lines can support the development of new microbial inoculants based on native strains such as GIBI029, adapted to local conditions. Future work should also consider scale-up, field validation, and transfer of the technology to farmers in order to achieve practical and sustainable solutions for horticultural production systems.

5. Conclusions

The native Colombian isolate G. diazotrophicus GIBI029 improved soil fertility and foliar nutrient status more effectively than the reference strain ATCC 49037 under greenhouse tomato production. Inoculation with GIBI029 coincided with higher soil organic matter and nutrient (N, P, K, Ca) levels and increased foliar N; these observations suggest improved overall nutrient availability under this treatment. These improvements were associated with higher tomato productivity and superior economic performance, demonstrating that strain origin is a critical factor influencing the agronomic effectiveness of microbial inoculants. The results highlight the potential of locally adapted bacterial isolates to contribute to more sustainable and profitable tomato production systems.
Future studies should validate these findings under commercial field conditions and over multiple growing seasons, as well as investigate the biological mechanisms underlying soil nutrient dynamics, plant nutrient uptake, and interactions between inoculated strains and native microbial communities. Therefore, the present results provide a useful basis for confirming the consistency of the observed responses and for supporting the future application of this technology in commercial tomato production.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/agriculture16141493/s1, Table S1: Initial soil chemical properties and their agronomic classification according to reference values for agricultural crops under controlled conditions, Table S2: Comparison of exchangeable bases and cationic ratios in the initial soil sample to theoretical levels for agricultural crops under controlled conditions, Table S3: Analysis of variance of the effect of four fertilization levels with nitrogen and phosphorus and the application of G. diazotrophicus on soil nutrient elements in greenhouse-grown tomato, Table S4: Analysis of variance of the effect of the macroelements on the content of nitrogen, protein, potassium, phosphorus, moisture, and dry matter in the foliar tissue of tomato according to the sources evaluated, and Table S5: Structure of production costs of the tomato crop with the application of the Colombian native G. diazotrophicus GIBI029 isolate as biofertilizer.

Author Contributions

Conceptualization, N.C.-A. and A.H.-S.; methodology, M.P. and J.A.C.; software, N.C.-A. and A.H.-S.; validation, G.M.R., N.C.-A., and A.H.-S.; formal analysis, G.M.R., N.C.-A., A.H.-S. and Ó.J.S.; investigation, M.P. and J.A.C.; resources, G.M.R., N.C.-A. and Ó.J.S.; data curation, N.C.-A. and G.M.R.; writing—original draft preparation, A.H.-S., M.P., J.A.C. and Ó.J.S.; writing—review and editing, A.H.-S. and Ó.J.S.; visualization, M.P. and J.A.C.; supervision, N.C.-A. and G.M.R.; project administration, G.M.R.; funding acquisition, G.M.R. and Ó.J.S. All authors have read and agreed to the published version of the manuscript.

Funding

This article is derived from the program “Biofactories: An Opportunity for Bioeconomic Development for Caldas through Biotechnology”, code 1235-903-8697, funded by the Colombian Ministry of Science, Technology and Innovation through the Francisco José de Caldas fund, contingent recovery contract No. 80740-503-2021, executed by the Universidad de Manizales in partnership with the Universidad de Caldas, Universidad Católica de Manizales, Universidad Católica Luis Amigó, Universidad Autónoma de Manizales, Gobernación de Caldas, Fundación Centro Internacional de Educación y Desarrollo Humano (CINDE), and Centro de Bioinformática y Biología Computacional de Colombia (BIOS). This research was also funded by the Universidad de Caldas and the Universidad Católica de Manizales through the research initiative “Production of a biofertilizer based on Gluconacetobacter diazotrophicus on the pilot scale and its evaluation in promoting the growth of vegetable crops”. The APC was funded by the Vice-rectorate for Research and Graduate Studies of the Universidad de Caldas.

Data Availability Statement

The data that support the findings of this study are available from the corresponding author upon reasonable request.

Acknowledgments

The authors thank the technical support of the Tesorito Farm at the Universidad de Caldas and the Research Institute in Microbiology and Agro-industrial Biotechnology at the Universidad Católica de Manizales. The administrative support of the Universidad de Manizales is acknowledged as well. The authors also acknowledge the use of ChatGPT (OpenAI, San Francisco, CA, USA; GPT-5.5 version) as an AI-based language assistance tool for translating the original Spanish manuscript into English and for improving the clarity, grammar, and overall academic writing of the manuscript. All scientific content, interpretations, and conclusions were developed and verified by the authors.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Compant, S.; Samad, A.; Faist, H.; Sessitsch, A. A review on the plant microbiome: Ecology, functions, and emerging trends in microbial application. J. Adv. Res. 2019, 19, 29–37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Santos, L.F.; Olivares, F.L. Plant microbiome structure and benefits for sustainable agriculture. Curr. Plant Biol. 2021, 26, 100198. [Google Scholar] [CrossRef] [Scilit]
  3. Khan, N.; Humm, E.A.; Jayakarunakaran, A.; Hirsch, A.M. Reviewing and renewing the use of beneficial root and soil bacteria for plant growth and sustainability in nutrient-poor, arid soils. Front. Plant Sci. 2023, 14, 1147535. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Hanif, M.S.; Tayyab, M.; Baillo, E.H.; Islam, M.M.; Islam, W.; Li, X. Plant microbiome technology for sustainable agriculture. Front. Microbiol. 2024, 15, 1500260. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Santoyo, G. How plants recruit their microbiome? New insights into beneficial interactions. J. Adv. Res. 2022, 40, 45–58. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Cavalcante, V.A.; Döbereiner, J. A new acid-tolerant nitrogen-fixing bacterium associated with sugar cane. Plant Soil 1988, 108, 23–31. [Google Scholar] [CrossRef] [Scilit]
  7. Schwister, E.M.; Dietz, B.R.; Knutson, C.M.; Olszewski, N.E.; Barney, B.M. Gluconacetobacter diazotrophicus gene fitness during diazotrophic growth. Appl. Environ. Microbiol. 2022, 88, e01241-22. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Dietz, B.R.; Olszewski, N.E.; Barney, B.M. Enhanced extracellular ammonium release in the plant endophyte Gluconacetobacter diazotrophicus through genome editing. Microbiol. Spectr. 2024, 12, e02478-23. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Delaporte-Quintana, P.; Grillo-Puertas, M.; Lovaisa, N.C.; Teixeira, K.R.; Rapisarda, V.A.; Pedraza, R.O. Contribution of Gluconacetobacter diazotrophicus to phosphorus nutrition in strawberry plants. Plant Soil 2017, 419, 335–347. [Google Scholar] [CrossRef] [Scilit]
  10. Delaporte-Quintana, P.; Lovaisa, N.C.; Rapisarda, V.A.; Pedraza, R.O. The plant growth promoting bacteria Gluconacetobacter diazotrophicus and Azospirillum brasilense contribute to the iron nutrition of strawberry plants through siderophores production. Plant Growth Regul. 2020, 91, 185–199. [Google Scholar] [CrossRef] [Scilit]
  11. Fernández-Delgado, J.; Abad-Rodríguez, E.M.; Salgado-Pulido, J.M. Efecto de Gluconacetobacter diazotrophicus en el cultivo del tomate (Solanum lycopercicum L.) (Efect of Gluconacetobacter diazotrophicus on tomato (Solanum lycopercicum L.) cultivation). Avances 2019, 21, 264–275. (In Spanish) [Google Scholar]
  12. Restrepo, G.M.; Ceballos, N.; Valencia, L.F.; Sánchez, Ó.J. Plant growth promotion by Gluconacetobacter diazotrophicus and its interaction with genotype and phosphorus availability in tomato seedlings. Org. Agr. 2021, 11, 601–614. [Google Scholar] [CrossRef] [Scilit]
  13. Restrepo, G.M.; Sánchez, Ó.J.; Marulanda, S.M.; Galeano, N.F.; Taborda, G. Evaluation of plant-growth promoting properties of Gluconacetobacter diazotrophicus and Gluconacetobacter sacchari isolated from sugarcane and tomato in West Central region of Colombia. Afr. J. Biotechnol. 2017, 16, 1619–1629. [Google Scholar] [CrossRef] [Scilit]
  14. Ceballos-Aguirre, N.; Hurtado-Salazar, A.; Restrepo, G.M.; Sánchez, Ó.J.; Hernández, M.C.; Montoya, M. Technical and economic assessment of tomato cultivation through a macro-tunnel production system with the application of Gluconacetobacter diazotrophicus. Horticulturae 2024, 10, 1110. [Google Scholar] [CrossRef] [Scilit]
  15. Ceballos-Aguirre, N.; Restrepo, G.M.; Patiño, S.; Cuéllar, J.A.; Sánchez, Ó.J. Utilization of Gluconacetobacter diazotrophicus in tomato crop: Interaction with nitrogen and phosphorus fertilization. Agriculture 2025, 15, 1191. [Google Scholar] [CrossRef] [Scilit]
  16. Kooshki, M.J.; Haghighi, M. Enhancing tomato growth, quality, and yield through the application of bio and nano-bio phosphorus in conjunction with Pseudomonas putida inoculation. J. Agric. Food Res. 2024, 18, 101483. [Google Scholar] [CrossRef] [Scilit]
  17. Huang, H.; Luo, D.; Chen, J.; Wang, T.; Zhang, Q.; Wang, Y. Effects of phosphorus-solubilizing bacteria on tomato seedling growth and soil phosphorus availability. J. Agro-Environ. Sci. 2025, 44, 3181–3189. [Google Scholar] [CrossRef]
  18. Shi, A.; Di, Q.; Xie, K.; Feng, X.; Wang, X.; Li, Y.; Sun, M.; Yu, X.; Wang, J.; Han, L. Tomato plant residues and Bacillus subtilis application can improve the soil environment and increase tomato yield and quality. Technol. Hortic. 2024, 4, e024. [Google Scholar] [CrossRef] [Scilit]
  19. Manzano-Gómez, L.A.; Rincón-Molina, C.I.; Martínez-Romero, E.; Stopol-Martínez, S.S.; Santos-Santiago, A.; Villalobos-Maldonado, J.J.; Ruíz-Valdiviezo, V.M.; Rincón-Rosales, R. Native rhizobial inoculation improves tomato yield and nutrient uptake while mitigating heavy metal accumulation in a conventional farming system. Microorganisms 2025, 13, 1904. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Han, Y.; Tian, L.; Luo, Y.; Han, L. Inoculation with PGPR co-fermented broths promotes growth, yields, and quality of pepper by increasing soil nutrients and changing soil bacterial community. J. Appl. Microbiol. 2024, 135, lxae289. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Ikiz, B.; Dasgan, H.Y.; Gruda, N.S. Utilizing the power of plant growth promoting rhizobacteria on reducing mineral fertilizer, improved yield, and nutritional quality of Batavia lettuce in a floating culture. Sci. Rep. 2024, 14, 1616. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Cazares-Esquivel, S.E.; Carballo-Sánchez, M.P.; Almaraz-Suárez, J.J. Effect of plant growth-promoting rhizobacteria on agronomic and macronutrient parameters in pak choi. Rev. Mex. Cienc. Agric. 2023, 14, 633–639. [Google Scholar] [CrossRef] [Scilit]
  23. Alzate Zuluaga, M.Y.; de Oliveira Caretta, T.; Agostini, A.; Monterisi, S.; Fattorini, R.; Cesco, S.; Pii, Y. Unlocking cucumber growth: Exploring the impact of nutrient availability levels and bacterial inoculation on plant growth and mineral composition. Hortic. Environ. Biotechnol. 2026, 67, 141–156. [Google Scholar] [CrossRef] [Scilit]
  24. Universidad de Caldas. Granja Tesorito (Tesorito Farm). Available online: https://cienciasagropecuarias.ucaldas.edu.co/granja-tesorito/ (accessed on 25 April 2024). (In Spanish)
  25. IUSS Working Group WRB. World Reference Base for Soil Resources. International Soil Classification System for Naming Soils and Creating Legends for Soil Maps; International Union of Soil Sciences: Vienna, Austria, 2022. [Google Scholar]
  26. Impulsores Internacionales SAS. Tomate Híbrido Roble 956 F1 (Roble 956 F1 Hybrid Tomato). Available online: https://www.impulsemillas.com/documentos/fichas/Toamate_Roble_compressed.pdf (accessed on 4 June 2024). (In Spanish)
  27. ImpulSemillas. Tomate Híbrido Roble 956 F1 (Roble 956 F1 Hybrid Tomato). Available online: https://www.impulsemillas.com/producto/tomate-roble-956-f1/ (accessed on 1 February 2022). (In Spanish)
  28. Jaramillo, J.E.; Sánchez, G.D.; Rodríguez, V.P.; Aguilar, P.A.; Gil, L.F.; Hío, J.C.; Pinzón, L.M.; García, M.C.; Quevedo, D.; Zapata, M.Á.; et al. Tecnología para el Cultivo de Tomate bajo Condiciones Protegidas (Technology for Tomato Cultivation Under Protected Conditions); Corpoica: Mosquera, Colombia, 2012. (In Spanish) [Google Scholar]
  29. Ceballos-Aguirre, N.; Cuellar, J.A.; Restrepo, G.M.; Sánchez, Ó.J. Effect of the application of Gluconacetobacter diazotrophicus and its interaction with nitrogen and phosphorus fertilization on carrot yield in the field. Int. J. Agron. 2023, 2023, 6899532. [Google Scholar] [CrossRef] [Scilit]
  30. Kimel de Colombia. Manual Técnico de Fertilizantes (Technical Fertilizer Manual); Kimel de Colombia: Bogotá, Colombia, 2012; pp. 8–11. (In Spanish) [Google Scholar]
  31. ICONTEC. Norma Técnica Colombiana NTC 5264. Calidad del suelo. Determinación del pH (Colombian Technical Standard NTC 5264. Soil Quality. Determination of pH); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2018; 11p. (In Spanish) [Google Scholar]
  32. ICONTEC. Norma Técnica Colombiana NTC 5403. Calidad del Suelo. Determinación del Carbono Orgánico (Colombian Technical Standard NTC 5403. Soil Quality. Determination of Organic Carbon); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2021; 18p. (In Spanish) [Google Scholar]
  33. DeBolt, D.C. A high sample volume procedure for the colorimetric determination of soil organic matter. Commun. Soil Sci. Plant Anal. 1974, 5, 131–137. [Google Scholar] [CrossRef] [Scilit]
  34. Bremner, J. Determination of nitrogen in soil by the Kjeldahl method. J. Agric. Sci. 1960, 55, 11–33. [Google Scholar] [CrossRef] [Scilit]
  35. ICONTEC. Norma Técnica Colombiana NTC 5350. Calidad del Suelo. Determinación de Fósforo Disponible (Colombian Technical Standard NTC 5350. Soil Quality. Determination of Available Phosphorus); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2020; 18p. (In Spanish) [Google Scholar]
  36. Bray, R.H.; Kurtz, L.T. Determination of total, organic, and available forms of phosphorus in soils. Soil Sci. 1945, 59, 39–46. [Google Scholar] [CrossRef] [Scilit]
  37. ICONTEC. Norma Técnica Colombiana NTC 5349. Calidad del Suelo. Determinación de las Bases Cambiables. Método del Acetato Amonio 1M, pH 7,0 (Colombian Technical Standard NTC 5349. Soil Quality. Determination of Exchangeable Bases. Method of Extraction Using Ammonium Acetate 1M and pH 7.0); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2016; 9p. (In Spanish) [Google Scholar]
  38. Gillman, G.P.; Bruce, R.C.; Davey, B.G.; Kimble, J.M.; Searle, P.L.; Skjemstad, J.O. A comparison of methods used for determination of cation exchange capacity. Commun. Soil Sci. Plant Anal. 1983, 14, 1005–1014. [Google Scholar] [CrossRef] [Scilit]
  39. ICONTEC. Norma Técnica Colombiana NTC 5526. Calidad del Suelo. Determinación de Micronutrientes Disponibles: Cobre, Zinc, Hierro y Manganeso (Colombian Technical Standard NTC 5526. Soil Quality. Determination of Available Micronutrients: Cupper, Zinc, Iron and Manganese); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2024; 11p. (In Spanish) [Google Scholar]
  40. Alvarez, J.M.; Lopez-Valdivia, L.M.; Novillo, J.; Obrador, A.; Rico, M.I. Comparison of EDTA and sequential extraction tests for phytoavailability prediction of manganese and zinc in agricultural alkaline soils. Geoderma 2006, 132, 450–463. [Google Scholar] [CrossRef] [Scilit]
  41. ICONTEC. Norma Técnica Colombiana NTC 5402. Calidad del suelo. Determinación del Azufre Disponible (Colombian Technical Standard NTC 5402. Soil Quality. Determination of Available Sulfur); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2006; 7p. (In Spanish) [Google Scholar]
  42. ICONTEC. Norma Técnica Colombiana NTC 5404. Calidad del Suelo. Determinación de Boro (Colombian Technical Standard NTC 5404. Soil quality. Determination of Boron); Instituto Colombiano de Normas Técnicas y Certificación (ICONTEC): Bogotá, Colombia, 2011; 8p. (In Spanish) [Google Scholar]
  43. John, K.M.; Chuah, H.H.; Neufeld, J.H. Application of improved Azomethine-H method to the determination of boron in soils and plants. Anal. Lett. 1975, 8, 559–568. [Google Scholar] [CrossRef] [Scilit]
  44. DANE. Boletín Semanal Precios Mayoristas (Weekly Wholesale Price Bulletin). Available online: https://www.dane.gov.co/index.php/estadisticas-por-tema/agropecuario/sistema-de-informacion-de-precios-sipsa/mayoristas-boletin-semanal-1 (accessed on 4 April 2024). (In Spanish)
  45. Corabastos. Boletín de Precios Diarios (Daily Price Bulletin). Available online: https://corabastos.com.co/boletin-precios-corabastos (accessed on 16 April 2024). (In Spanish)
  46. Ceballos-Aguirre, N.; Restrepo, G.M.; Hurtado-Salazar, A.; Cuellar, J.A.; Sánchez, Ó.J. Economic feasibility of Gluconacetobacter diazotrophicus in carrot cultivation. Rev. Ceres 2022, 69, 40–47. [Google Scholar] [CrossRef] [Scilit]
  47. Barrow, N.; Hartemink, A.E. The effects of pH on nutrient availability depend on both soils and plants. Plant Soil 2023, 487, 21–37. [Google Scholar] [CrossRef] [Scilit]
  48. Rietra, R.P.J.J.; Heinen, M.; Dimkpa, C.O.; Bindraban, P.S. Effects of nutrient antagonism and synergism on yield and fertilizer use efficiency. Commun. Soil Sci. Plant Anal. 2017, 48, 1895–1920. [Google Scholar] [CrossRef] [Scilit]
  49. Sánchez, G.P. Tablas Guía Para la Interpretación de Análisis de Suelos (Guide Tables for Soil Analysis Interpretation). Available online: https://es.scribd.com/document/458120256/TABLAS-GUIA-PARA-INTERPRETAR-ANALISIS-DE-SUELOS (accessed on 3 March 2024). (In Spanish)
  50. Weil, N.C.; Brady, R.R.; Weil, R.R. The Nature and Properties of Soils; Pearson: Columbus, OH, USA, 2016. [Google Scholar]
  51. Havlin, J.L.; Tisdale, S.L.; Nelson, W.L.; Beaton, J.D. Soil Fertility and Fertilizers; Pearson Education: Noida, India, 2016. [Google Scholar]
  52. Marschner, H. Marschner’s Mineral Nutrition of Higher Plants; Academic Press: Cambridge, MA, USA, 2011. [Google Scholar]
  53. Velásquez, G.; Calabi-Floody, M.; Poblete-Grant, P.; Rumpel, C.; Demanet, R.; Condron, L.; Mora, M. Fertilizer effects on phosphorus fractions and organic matter in Andisols. J. Soil Sci. Plant Nutr. 2016, 16, 294–309. [Google Scholar] [CrossRef] [Scilit]
  54. Hou, E.; Luo, Y.; Kuang, Y.; Chen, C.; Lu, X.; Jiang, L.; Luo, X.; Wen, D. Global meta-analysis shows pervasive phosphorus limitation of aboveground plant production in natural terrestrial ecosystems. Nat. Commun. 2020, 11, 637. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  55. Gao, W.; Zhao, J.; Guo, X.; Wang, F.; Chen, X.; Zhu, Z.; Ge, T.; Wang, L.; Kuzyakov, Y.; Wu, J. Intensive N2 fixation accelerates microbial turnover in cropland soils. Sci. Total Environ. 2024, 916, 170081. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  56. Ruzzi, M.; Aroca, R. Plant growth-promoting rhizobacteria act as biostimulants in horticulture. Sci. Hortic. 2015, 196, 124–134. [Google Scholar] [CrossRef] [Scilit]
  57. Luna, M.F.; Aprea, J.; Crespo, J.M.; Boiardi, J.L. Colonization and yield promotion of tomato by Gluconacetobacter diazotrophicus. Appl. Soil Ecol. 2012, 61, 225–229. [Google Scholar] [CrossRef] [Scilit]
  58. Arbelaez, L.; Rivera, J.; Hurtado-Salazar, A.; Ceballos-Aguirre, N. Technical and economic evaluation of three types of tomato nutrient solutions under semi-controlled conditions. J. Agric. Sci. 2016, 8, 68–78. [Google Scholar] [CrossRef] [Scilit]
  59. Yadav, R.; Suman, A.; Prasad, S.; Prakash, O. Effect of Gluconacetobacter diazotrophicus and Trichoderma viride on soil health, yield and N-economy of sugarcane cultivation under subtropical climatic conditions of India. Eur. J. Agron. 2009, 30, 296–303. [Google Scholar] [CrossRef] [Scilit]
  60. Dent, D. Non-nodular endophytic bacterial symbiosis and the nitrogen fixation of Gluconacetobacter diazotrophicus. In Symbiosis; Rigobelo, E.C., Ed.; IntechOpen: London, UK, 2018; Volume 4, pp. 53–81. [Google Scholar]
  61. Farneselli, M.; Reale, L.; Falcinelli, B.; Akram, M.Z.; Cimarelli, S.; Cinti, E.; Paglialunga, M.; Carbone, F.; Pannacci, E.; Tei, F. A multifaceted approach to optimizing processed tomato production: Investigating the combined effects of biostimulants and reduced nitrogen fertilization. Horticulturae 2025, 11, 931. [Google Scholar] [CrossRef] [Scilit]
  62. Richardson, A.E.; Simpson, R.J. Soil microorganisms mediating phosphorus availability update on microbial phosphorus. Plant Physiol. 2011, 156, 989–996. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  63. Jiang, J.; Wang, Y.-P.; Yang, Y.; Yu, M.; Wang, C.; Yan, J. Interactive effects of nitrogen and phosphorus additions on plant growth vary with ecosystem type. Plant Soil 2019, 440, 523–537. [Google Scholar] [CrossRef] [Scilit]
  64. Guilherme, E.A.; Nascimento, C.S.; Lobo, A.K.M.; Carvalho, F.E.L.; Silveira, J.A.G. Nitrogen-utilization efficiency during early deficiency after a luxury consumption is improved by sustaining nitrate reductase activity and photosynthesis in cotton plants. Plant Soil 2019, 443, 185–198. [Google Scholar] [CrossRef] [Scilit]
  65. Saravanan, V.; Madhaiyan, M.; Osborne, J.; Thangaraju, M.; Sa, T. Ecological occurrence of Gluconacetobacter diazotrophicus and nitrogen-fixing Acetobacteraceae members: Their possible role in plant growth promotion. Microb. Ecol. 2008, 55, 130–140. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  66. Mamani-Rojas, L.; Rengifo, R.; Velarde-Apaza, L.; Ramírez-Rojas, M.; Cántaro-Segura, H. Biocontrol and plant growth-promoting potential of Bacillus and Actinomycetes isolated from the rhizosphere and phyllosphere of Potato (Solanum tuberosum L.) from different agroecological zones of Peru. Appl. Microbiol. 2026, 6, 2. [Google Scholar] [CrossRef] [Scilit]
  67. Aasfar, A.; Bargaz, A.; Yaakoubi, K.; Hilali, A.; Bennis, I.; Zeroual, Y.; Meftah Kadmiri, I. Nitrogen fixing Azotobacter species as potential soil biological enhancers for crop nutrition and yield stability. Front. Microbiol. 2021, 12, 628379. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  68. Padwar, G.; Padwar, G.K.; Dubey, S. Studies on stover yield of maize with basal application of fertilizer and foliar spraying of Gluconacetobacter diazotropicus on available nutrients in soil. Int. J. Plant Soil Sci. 2023, 35, 232–238. [Google Scholar] [CrossRef] [Scilit]
  69. Pellegrini, M.; Pagnani, G.; Rossi, M.; D’Egidio, S.; Gallo, M.D.; Forni, C. Daucus carota L. seed inoculation with a consortium of bacteria improves plant growth, soil fertility status and microbial community. Appl. Sci. 2021, 11, 3274. [Google Scholar] [CrossRef] [Scilit]
  70. Murumkar, D.; Nalawade, S.; Indi, D.; Pawar, S. Response of sugarcane seed plot to microbial inoculation by Gluconacetobacter diazotrophicus and phosphate-solubilizing bacteria. Sugar Tech 2017, 19, 26–32. [Google Scholar] [CrossRef] [Scilit]
  71. Chawla, N.; Phour, M.; Suneja, S.; Sangwaan, S.; Goyal, S. Gluconacetobacter diazotrophicus: An overview. Res. Environ. Life Sci. 2014, 7, 1–10. [Google Scholar]
  72. Pellegrini, M.; Spera, D.; Ercole, C.; del Gallo, M. Allium cepa L. seed inoculation with a consortium of plant growth-promoting bacteria: Effects on plant growth and development and soil fertility status and microbial community. In Proceedings of the 1st International Electronic Conference on Microbiology, Basel, Switzerland, 2–30 November 2020. [Google Scholar]
  73. Fallah, N.; Yang, Z.; Tayyab, M.; Zhang, C.; Abubakar, A.Y.; Lin, Z.; Pang, Z.; Allison, A.; Zhang, H. Depth-dependent influence of biochar application on the abundance and community structure of diazotrophic under sugarcane growth. PLoS ONE 2021, 16, e0253970. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  74. Yan, J.; Han, X.; Lu, X.; Chen, X.; Zou, W. Land use indirectly affects the cycling of multiple nutrients by altering the diazotrophic community in black soil. J. Sci. Food Agric. 2022, 102, 3788–3795. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  75. Shukla, S.; Sharma, L.; Jaiswal, V.; Pathak, A.; Tiwari, R.; Awasthi, S.; Gaur, A. Soil quality parameters vis-a-vis growth and yield attributes of sugarcane as influenced by integration of microbial consortium with NPK fertilizers. Sci. Rep. 2020, 10, 19180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Location of the experimental site at Tesorito Experimental Farm, Universidad de Caldas, Manizales, Colombia. Satellite image and map of the experimental facilities indicating the two greenhouses used in this study. The map was prepared by the authors using Google Earth Pro version 10.110.84.2 (Google LLC, Mountain View, CA, USA).
Agriculture 16 01493 g001
Figure 2. Effect of N and P fertilizer addition and two G. diazotrophicus strains on mineral elements in a tomato-cultivated soil 180 days after transplanting under controlled conditions. (a) Edaphic content of N and organic matter; (b) edaphic concentrations of K, Ca, Mg, Na, and P. Different lowercase letters indicate significant differences among treatments according to Duncan’s multiple-range test (p < 0.05). AT: ATCC 49037 strain; GB: native GIBI029 isolate; OM: organic matter. Codes are deciphered in Table 1.
Agriculture 16 01493 g002
Figure 3. Foliar nutrient content of N, K, and P in tomato plants at 160 days after transplanting as influenced by N and P fertilization and inoculation with two G. diazotrophicus strains under controlled conditions. Different lowercase letters indicate significant differences among treatments according to Duncan’s multiple-range test (p < 0.05). AT: ATCC 49037 strain; GB: native GIBI029 isolate.
Agriculture 16 01493 g003
Figure 4. Correlation heatmap representing the relationships among soil chemical properties and foliar variables in tomato plants under different treatments. Positive correlations are shown in blue and negative correlations in red. The matrix integrates edaphic and foliar interactions, highlighting key associations such as the strong coupling between organic matter and N and the antagonistic relationships affecting nutrient balance at the plant level. Values correspond to Pearson correlation coefficients ranging from −1 to +1, where the sign indicates the direction (positive or negative) and the magnitude indicates the strength of the relationship between variables.
Agriculture 16 01493 g004
Figure 5. Response surface illustrating the interaction effects of N, P, and K concentrations at the soil and foliar levels on yield. (a) N; (b) P; (c) K.
Agriculture 16 01493 g005
Table 1. Treatment combinations of the experimental setup.
MicroorganismConcentration
(CFU/mL)
N Fertilization
(%)
P Fertilization
(%)
Code
Native G. diazotrophicus GIBI029 isolate18 × 107100100100N100P-GB
Native G. diazotrophicus GIBI029 isolate18 × 1071000100N0P-GB
Native G. diazotrophicus GIBI029 isolate18 × 10701000N100P-GB
Native G. diazotrophicus GIBI029 isolate18 × 107000N0P-GB
G. diazotrophicus ATCC 49037 reference strain18 × 107100100100N100P-AT
G. diazotrophicus ATCC 49037 reference strain18 × 1071000100N0P-AT
G. diazotrophicus ATCC 49037 reference strain18 × 10701000N100P-AT
G. diazotrophicus ATCC 49037 reference strain18 × 107000N0P-AT
None0100100100N100P
None01000100N0P
None001000N100P
None0000N0P
Table 2. Exchangeable cationic relationships in soil at 180 days after transplanting tomato plants under controlled conditions, as influenced by the type of bacteria added, N, and P fertilization.
Treatments 1Ca2+/Mg2+Ca2+/K+Mg2+/K+K+/NO3Ca2+ + Mg2+/K+Ca2+ + Mg2+ + K+ + Na+Yield 2 (t/ha)
100N100P-GB2.8513.24.641.0917.913.7106.4
100N0P-GB2.925.51.882.647.414.598.0
0N100P-GB1.694.22.453.296.616.194.7
0N0P-GB2.402.10.897.343.020.1106.1
100N100P-AT2.536.32.482.098.813.144.8
100N0P-AT2.956.22.111.818.310.447.4
0N100P-AT3.213.81.173.414.912.041.5
0N0P-AT2.621.40.558.962.017.637.3
100N100P2.9618.26.140.824.311.960.2
100N0P2.825.82.072.387.912.155.9
0N100P2.542.71.063.223.89.646.8
0N0P2.021.00.489.271.413.256.7
1 Treatment codes are deciphered in Table 1. 2 Yield data for each treatment were taken from Ceballos-Aguirre et al. [15] from the same greenhouse experiment and under the same experimental conditions.
Table 3. Canonical correlation between foliar variables assessed in this study.
N
(g/kg)
Protein
(g/kg)
K
(g/kg)
P
(g/kg)
Moisture
(g/kg)
Dry Matter
(g/kg)
N
(g/kg)
10.12−0.30 ^−0.260.10−0.10
Protein
(g/kg)
0.125810.0140.14−0.170.17
K
(g/kg)
−0.30520.01410.54 *−0.100.10
P
(g/kg)
−0.26170.14130.53631−0.210.21
Moisture
(g/kg)
0.0934−0.1735−0.0987−0.20581−1 *
Dry Matter
(g/kg)
−0.09340.17350.09870.2058−11
Ash
(g/kg)
−0.22830.22930.77420.4668−0.07680.0768
Values correspond to Pearson correlation coefficients ranging from −1 to +1, where the sign indicates the direction (positive or negative) and the magnitude indicates the strength of the relationship between variables. Statistically significant correlations are indicated by an asterisk (*) at p < 0.05. The symbol (^) denotes a trend toward association, indicating a moderate correlation that does not reach statistical significance but may suggest a biologically relevant relationship.
Table 4. Canonical correlation between edaphic variables assessed in this study.
OM
(g/kg)
N
(g/kg)
P
(mg/kg)
K
(cmol/kg)
Ca
(cmol/kg)
Mg
(cmol/kg)
Na
(cmol/kg)
OM
(g/kg)
10.99 *0.240.250.330.42−0.015
N
(g/kg)
0.997110.240.250.330.43−0.01
P
(mg/kg)
0.24530.24111−0.280.40 ^0.49 ^−0.35
K
(cmol/kg)
0.24920.2536−0.27661−0.030.200.51
Ca
(cmol/kg)
0.32890.33190.3962−0.031310.59 *0.25
Mg
(cmol/kg)
0.42150.43280.48750.19910.58711−0.05
Na
(cmol/kg)
−0.0149−0.011−0.35310.50860.2485−0.05381
Values correspond to Pearson correlation coefficients ranging from −1 to +1, where the sign indicates the direction (positive or negative) and the magnitude indicates the strength of the relationship between variables. Statistically significant correlations are indicated by an asterisk (*) at p < 0.05. The symbol (^) denotes a trend toward association, indicating a moderate correlation that does not reach statistical significance but may suggest a biologically relevant relationship.
Table 5. Economic analysis of tomato production: Influence of N and P fertilization and G. diazotrophicus inoculation under semi-controlled conditions.
TreatmentGross Income
(USD/ha)
Cost per Hectare
(USD/ha)
UPM
(USD/kg)
Net Income
(USD/ha)
B/C
100N100P-GB32,37014,1100.1318,2592.29
100N0P-GB29,81413,3320.1416,4822.24
0N100P-GB28,81013,1600.1415,6502.19
0N0P-GB32,27812,1720.1120,1062.65
100N100P-AT13,62914,1100.31−4810.97
100N0P-AT14,42013,3320.2710881.08
0N100P-AT12,62513,1600.32−5350.96
0N0P-AT11,34812,1720.33−8250.93
100N100P18,31413,8670.2344471.32
100N0P17,00613,0890.2339171.3
0N100P14,23812,9170.2813211.1
0N0P17,25011,9290.2153201.45
B/C: benefit/cost ratio; UPM: unit production margin.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.