


Abstract
The endocannabinoid system (ECS) plays an integral role in maintaining metabolic homeostasis and may affect hunger, caloric intake, and nutrient absorption. Obesity has been associated with higher levels of the endogenous cannabinoid transmitters (endocannabinoids). Therefore, the ECS is an important target in obesity treatment. Modulating the enzymes that synthesize and degrade endocannabinoids, namely fatty acid amide hydrolase (FAAH), monoacylglycerol lipase (MAGL), and diacylglycerol lipase (DAGL), may be a promising strategy to treat obesity. This review aims to synthesize all studies investigating pharmacological or genetic manipulation of FAAH, MAGL, or DAGL enzymes in association with obesity-related measures. Pharmacological inhibition or genetic deletion of FAAH tended to promote an obesogenic state in animal models, though the relationships between human FAAH polymorphisms and obesity-related outcomes were heterogeneous, which could be due to FAAH having both pro-appetitive and anti-appetitive substrates. Genetic deletion of Mgll and Dagla as well as pharmacological inhibition of DAGL tended to reduce body weight and improve metabolic state in animal studies, though the effects of Mgll manipulation were tissue-dependent. Monitoring changes in body weight in ongoing clinical trials of FAAH inhibitors may clarify whether FAAH inhibition is a potential therapeutic strategy for treatment obesity. More preclinical work is needed to characterize the role of MAGL and DAGL modulation in obesity-related outcomes.
1. Introduction
Obesity is a significant and ever-growing public health concern defined by a body mass index (BMI) of greater than 30 kg/m2. Global data indicate that age-standardized obesity rates rose from 3.2% in 1975 to 10.8% in 2014 for men and from 6.4% in 1975 to 14.9% in 2014 for women [1]. The latest data from the NCD Risk Factor Collaboration showed that in 2016, almost 2 billion adults (39% of the global adult population) were estimated to be overweight (BMI ≥ 25 kg/m2) and 671 million (12% of the global adult population) had obesity [2]. Obesity has been associated with numerous adverse health outcomes, including increased incidence of type II diabetes, cancers, and cardiovascular disease [3], and has both direct (medical) and indirect (nonmedical) costs that pose a significant global economic burden [4]. Developing effective therapeutic strategies to treat obesity is thus a global health priority.
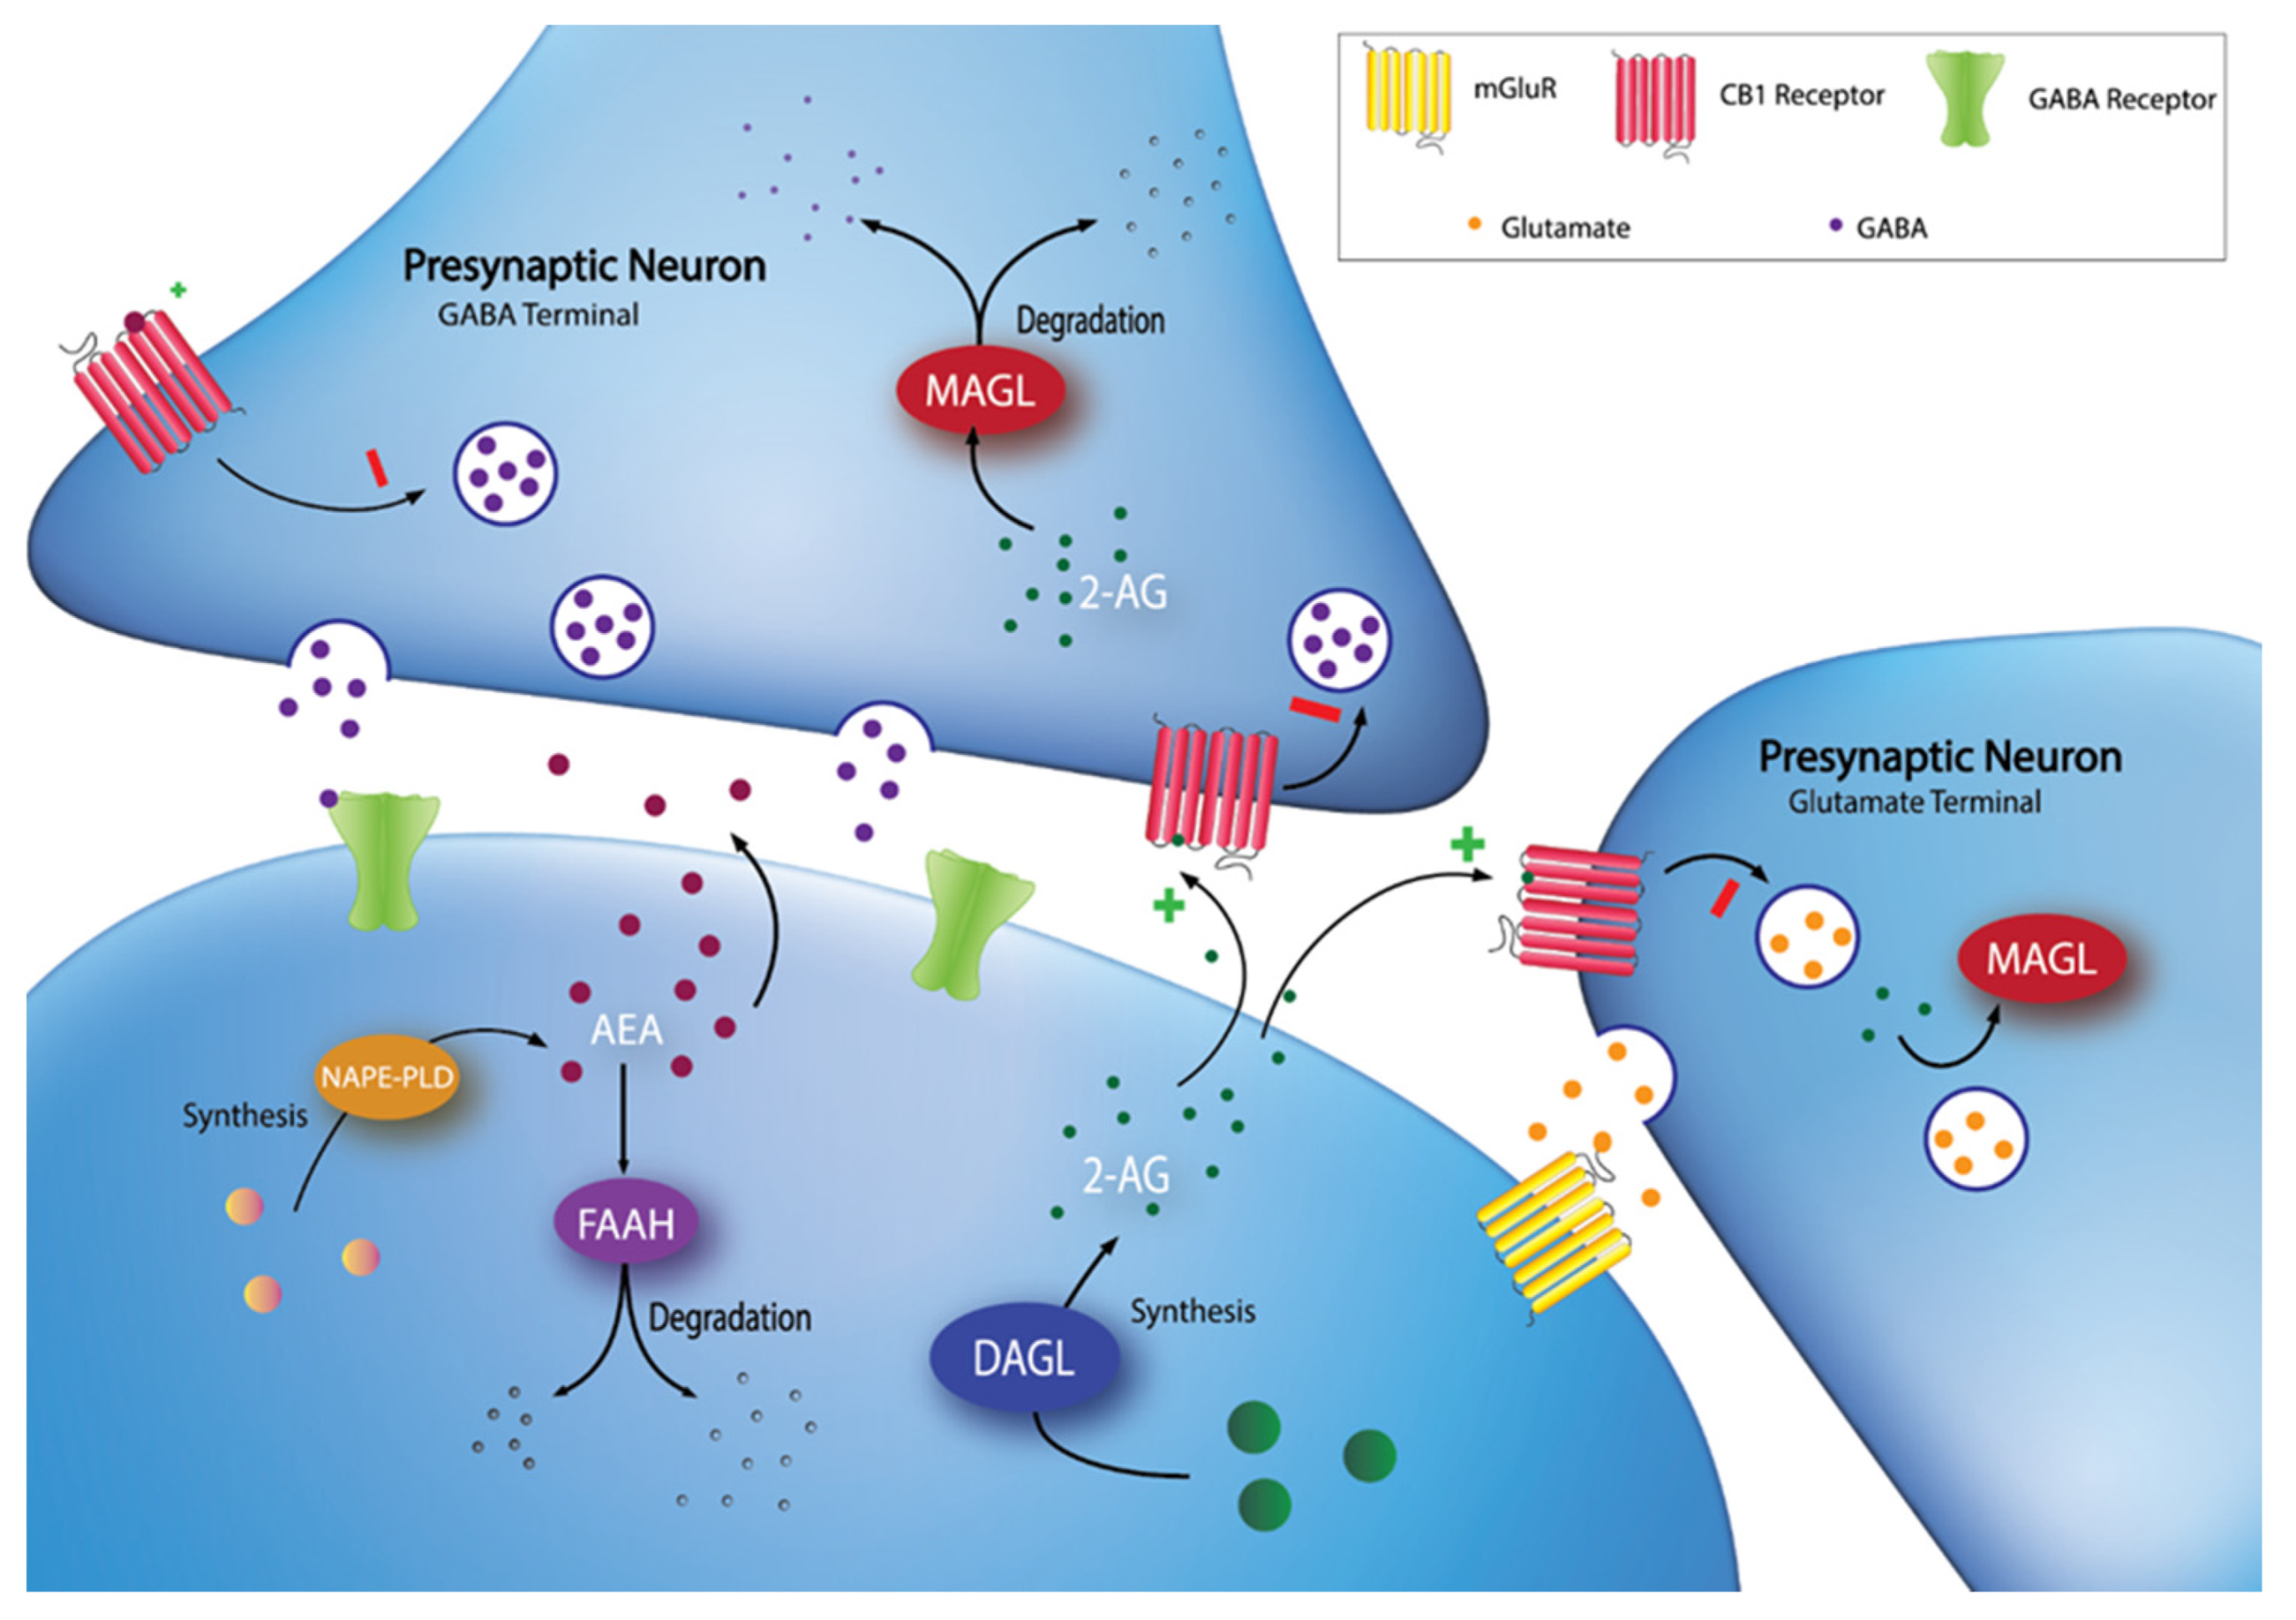
The endocannabinoid system (ECS) was recognized as a potential target for obesity treatment in the early 2000’s [5]. The ECS is an evolutionarily conserved lipid signalling system that has widespread involvement in nearly all physiological processes, including energy homeostasis, synaptic plasticity, and feeding behaviours [6]. The major components of the ECS include: two canonical G-protein coupled receptors, the cannabinoid type-1 (CB1) and type-2 (CB2) receptors; the endogenous ligands (endocannabinoids), which are phospholipid derivatives containing a poly-unsaturated fatty acid moiety and a polar head group, either ethanolamine in the case of arachidonoylethanolamide (anandamide; AEA) or glycerol in the case of 2-arachidonoylglycerol (2-AG); and the enzymes responsible for the synthesis and degradation of the endocannabinoids [7]. One major synthetic pathway for 2-AG involves the enzyme diacylglycerol lipase (DAGL), while AEA synthesis is more varied [6]. DAGL has two isoforms, DAGLα and DAGLβ, which are encoded by two different human genes, DAGLA and DAGLB [8]. In terms of degradation, fatty acid amide hydrolase (FAAH), encoded by the human FAAH gene, is one of the most studied ECS enzymes, as it is responsible for the majority of AEA metabolism and is involved to a lesser extent in 2-AG metabolism [7]. Similarly, monoacylglycerol lipase (MAGL), encoded by the human MGLL gene, is responsible for the majority of 2-AG metabolism [7]. See Figure 1 for an overview of the ECS.
Figure 1.
Synaptic localization of endocannabinoid synthesis and degradation. 2-AG is synthesized on-demand in the postsynaptic neuron by DAGL. Following synthesis, 2-AG diffuses into the synaptic cleft and activates CB1 receptors at GABA and glutamate terminals. 2-AG signaling can be terminated by MAGL degradation in the presynaptic terminal. AEA can be synthesized through multiple pathways (e.g., through a pathway involving NAPE-PLD), then diffuses into the synapse to activate CB1 receptors. Extracellular AEA undergoes reuptake into the postsynaptic cell and is hydrolyzed by FAAH.
The ECS has a multi-faceted role in the control of food intake and body weight, and it acts through both peripheral and central mechanisms. In the periphery, activation of CB1 receptors (e.g., by binding of AEA or 2-AG) promotes fat storage in adipocytes and increases lipogenesis, increases glucose uptake, and reduces satiety signals [9]. Centrally, activation of the ECS interferes with the control of hunger and satiety in multiple brain regions, including the hypothalamus and brain stem [9]. This likely involves a complex interplay between endocannabinoids and other neurotransmitters or hormones involved in hunger and satiety such as cholecystokinin (CCK), glucagon-like peptide 1 (GLP-1), and neuropeptide Y (NPY) [9]. Since the primary physiological function of the ECS is thought to shift energy balance towards energy storage, overactivation of the ECS likely contributes to obesity [5]. Numerous studies have found a positive association between circulating levels of endocannabinoids (AEA and/or 2-AG) and obesity in humans [10,11,12]. The elevated levels of endocannabinoids in human obesity are related to diet [13] and have been found to decrease after bariatric surgery [14].
Given that activation of the ECS increases food intake and energy storage, and that excessive activation of the ECS contributes to the pathogenesis of obesity, antagonism of the ECS has been explored as a potential therapeutic strategy [5,15]. In the early to mid-2000’s, the multi-center Rimonabant in Obesity (RIO) trials found significant evidence that rimonabant, a CB1 receptor antagonist/inverse agonist, reduced body weight in adults with obesity, and improved other secondary measures such as dyslipidemia and cardiometabolic risk factors [16,17]. Unfortunately, the promise of rimonabant as an obesity treatment was short-lived, as it was withdrawn from the market due to mounting evidence of serious psychiatric adverse effects, including increased risk of suicidal ideation and depression [18,19,20]. The promise of rimonabant to treat obesity led to efforts to develop and test numerous other CB1 receptor ligands that might have potential to modulate body weight and treat obesity. Interested readers are directed to our previous review of CB1 receptor ligands and their potential to treat obesity [15]. In brief, some potential strategies to target the CB1 receptor without producing serious psychiatric adverse effects include peripherally-restricted CB1 inverse agonists, CB1 receptor partial agonists, and CB1 receptor neutral antagonists.
Rather than directly targeting the CB1 receptor, another potential strategy to modulate ECS activity is to target the enzymes responsible for synthesis and/or degradation of the endocannabinoids. Two approaches can be undertaken: (1) targeting endocannabinoid degradation, i.e., by inhibiting FAAH or MAGL, and (2) targeting endocannabinoid biosynthesis, i.e., by inhibiting DAGL or another synthetic enzyme [8]. Given that obesity is associated with enhanced endocannabinoid tone, inhibiting endocannabinoid biosynthesis (e.g., with a DAGL inhibitor) is the most biologically plausible approach. However, the activity of ECS enzymes is complex, so it is hard to predict the effect of inhibiting ECS enzymes. For example, in some tissues FAAH inhibition may target 2-AG in addition to AEA, and it can both increase and decrease 2-AG concentrations [21]. There are also other substrates of FAAH that have a role in metabolism and satiety such as oleoylethanolamine (OEA) and palmitoylethanoamine (PEA). OEA is notable in particular as it has been shown to reduce food intake and suppress appetite, which is opposite to the effects of the endocannabinoids [22]. As FAAH metabolizes both pro-appetitive and anti-appetitive lipids, inhibition of FAAH would be expected to have mixed effects on appetite and body weight. It should be also noted that AEA and 2-AG have complex regulations; for example, AEA has been shown to inhibit metabolism and actions of 2-AG in the striatum [23].
To date, previous reviews have highlighted the genetic association between variation in the FAAH gene and obesity-related outcomes in humans [9,24]. However, no previous reviews have focused specifically on evidence for a potential role of ECS enzymes in obesity treatment. Thus, the goal of the present review was to systematically review the published empirical literature and qualitatively synthesize existing evidence that either pharmacological or genetic manipulation/variation of FAAH, MAGL, and DAGL might impact obesity-related outcomes. Since the published literature we identified for the present review was so heterogeneous in study design and outcomes, we decided to present this as a narrative review.
2. Search Strategy
A search was conducted on 13 July 2021 in the PubMed database. The following terms were used in a Boolean search format: (FAAH OR “Fatty acid amide hydrolase” OR MAGL OR MGL OR “Monoacylglycerol lipase” OR DAGL OR DGL OR “Diacylglycerol lipase”) AND (obesity). A single search was conducted that included both preclinical and clinical studies.
Inclusion of an article was determined on the basis of its design, intervention(s), and endpoint(s). In terms of design, only studies involving humans or animal models were included. With regards to intervention, the study needed to feature (1) administration of a FAAH, MAGL, or DAGL inhibitor AND/OR (2) investigation of genetic variation in FAAH, MGLL, or DAGLA genes. With either of these interventions, a connection to obesity-related endpoints was also necessary. Specifically, relevant endpoints included measures of (1) body weight or body mass index (BMI), (2) body fat composition or distribution, (3) food intake or feeding behaviour, (4) glycemic markers, and/or (5) lipid profiles. These endpoints were selected from a review on metabolic endpoints in animal models of obesity [25]. Studies were included only when the title and/or abstract made an explicit mention of obesity, body weight, or related endpoints.
A hierarchy of exclusion criteria was also established. Studies were first excluded if they were written in the wrong language (i.e., not English). Next, studies were excluded on the basis of wrong study design. Common studies excluded under this criterion were review/non-empirical articles, in vitro studies, and genetic studies that did not consider variants or polymorphisms in the relevant genes. Studies were then excluded if they used the wrong intervention. Namely, this applied to pharmacological studies that did not administer a FAAH, MAGL, or DAGL inhibitor. Finally, studies were excluded if they did not measure an obesity-related outcome.
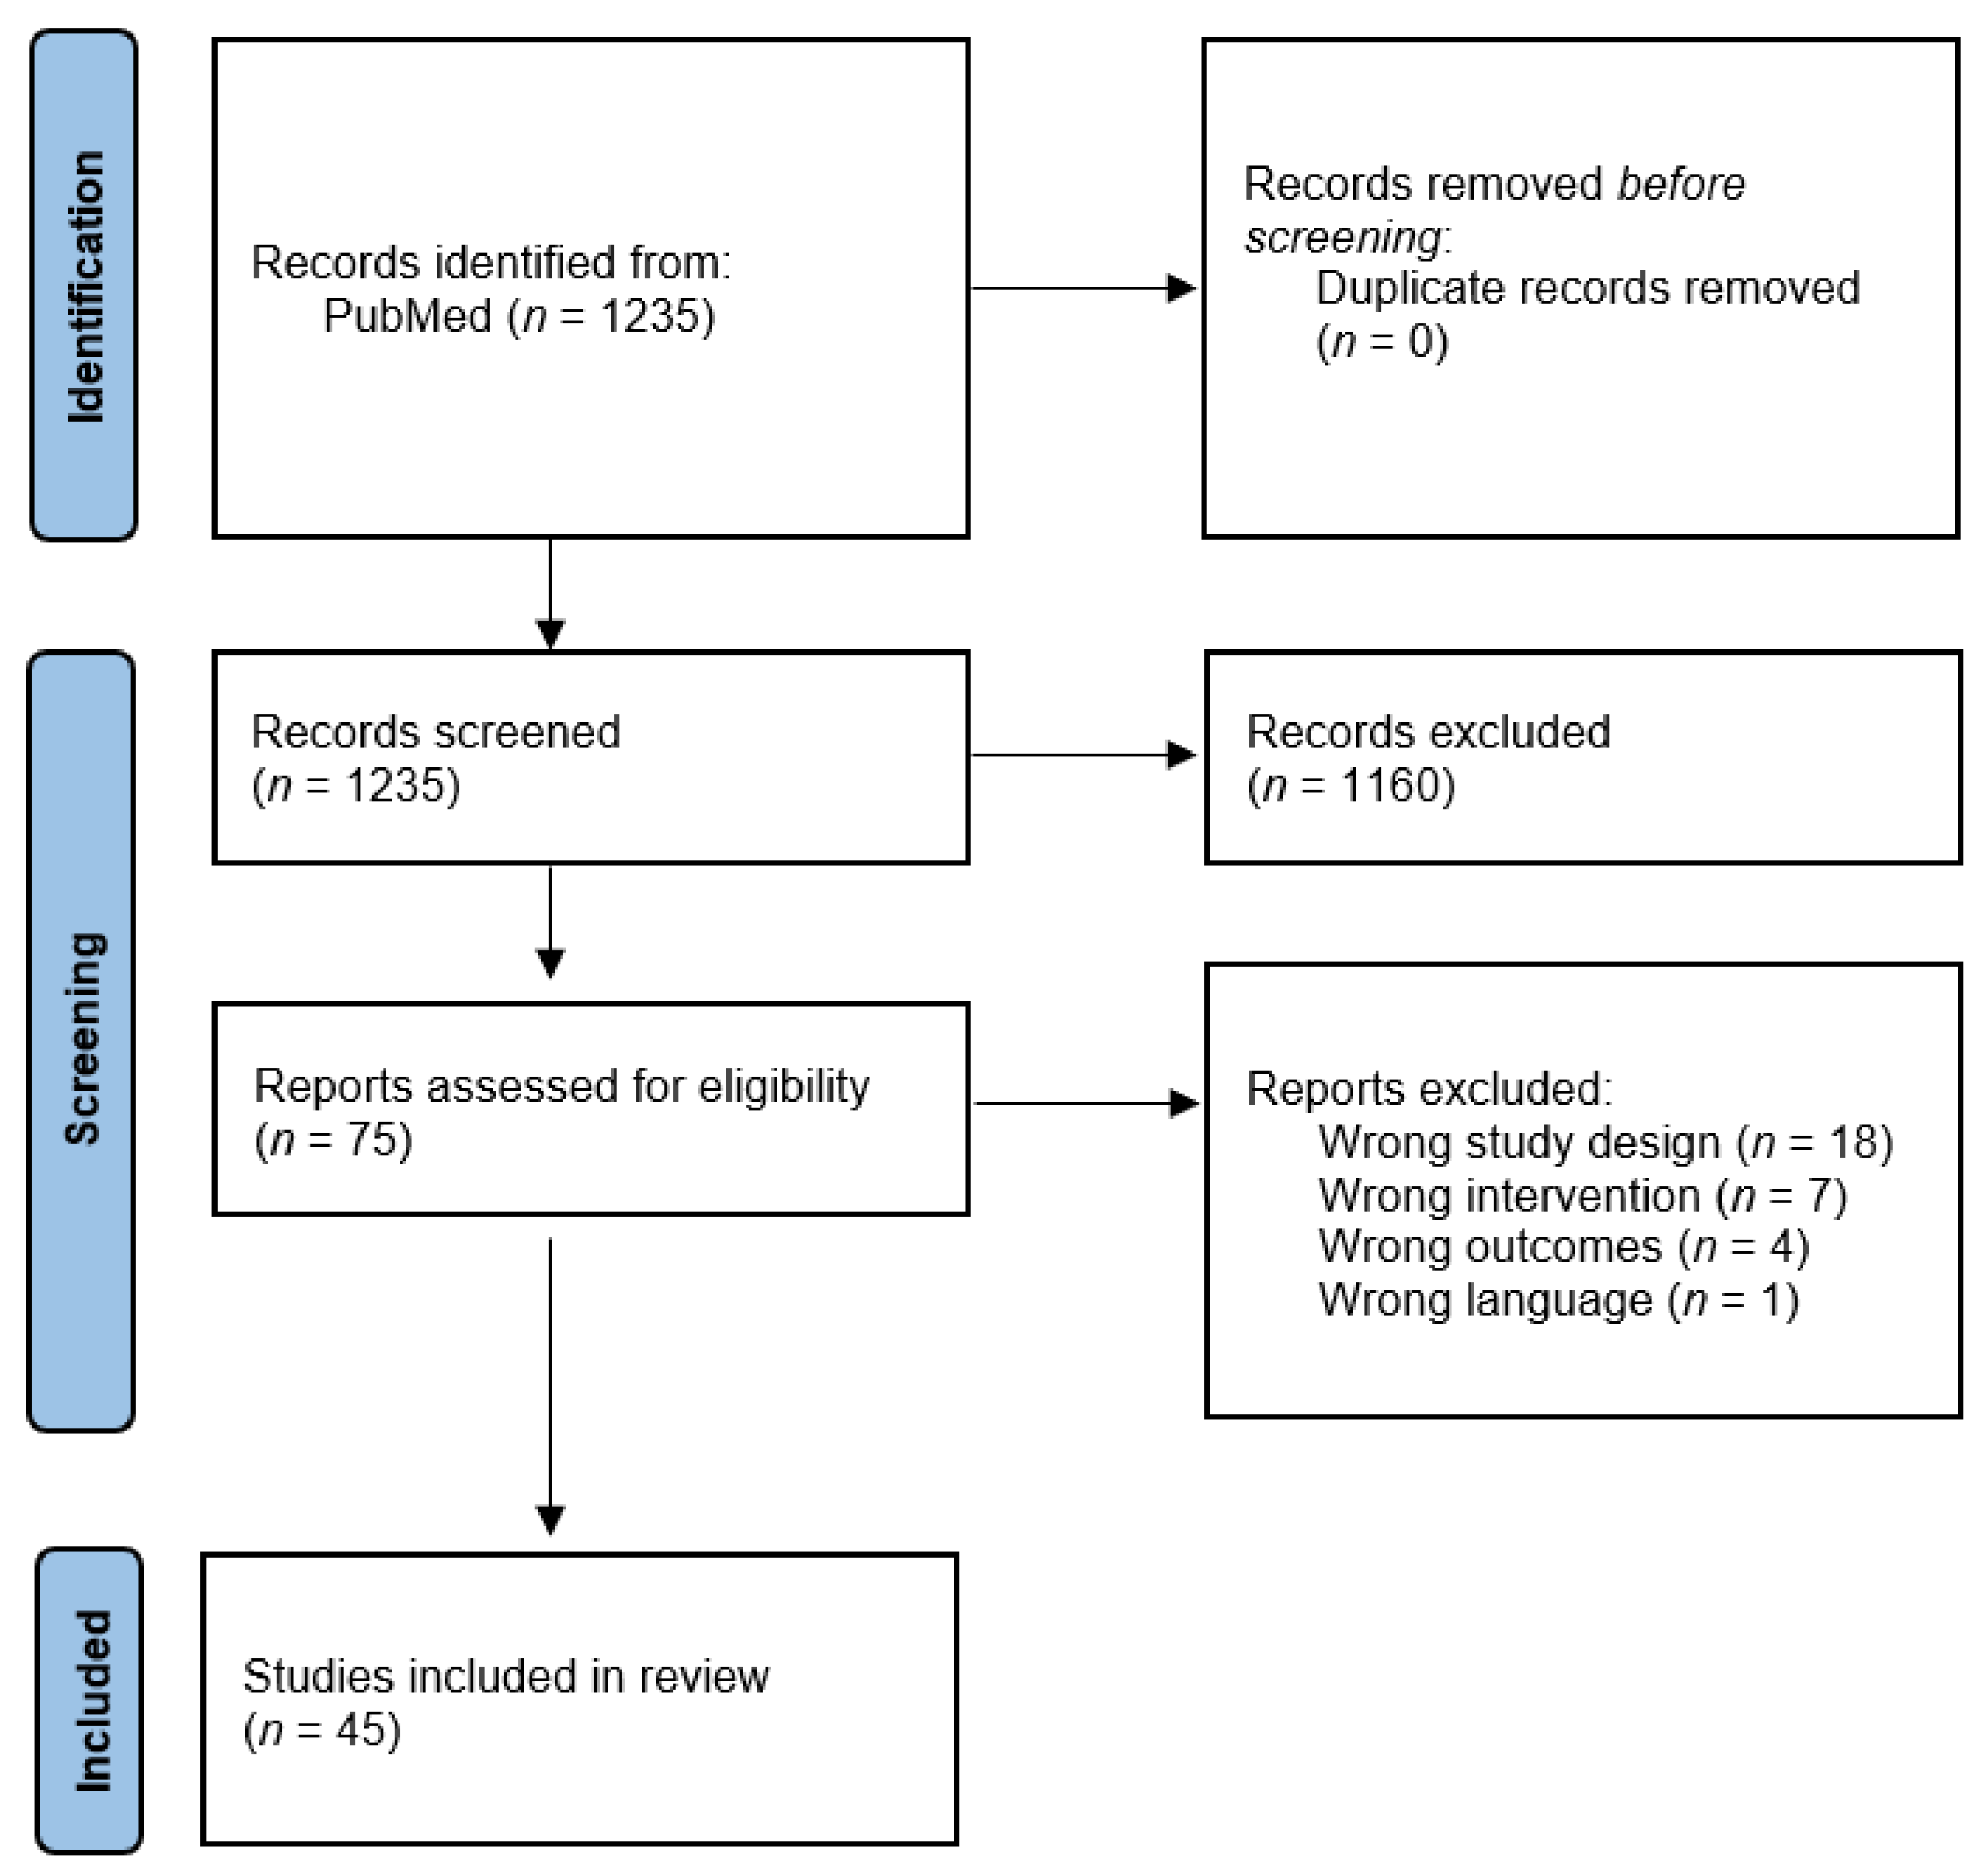
Figure 2 provides a Preferred Reporting Items for Systematic Reviews and Meta-Analyses (PRISMA) flowchart of the screening process for this review, conducted through Covidence. The initial search on July 13 produced 1235 studies from the PubMed database. During title and abstract screening, two reviewers were assigned to each article, and 1160 studies were removed. Seventy-five studies were left for full-text eligibility screening, and in this phase, 30 studies were excluded: 1 for wrong language, 18 for wrong study design, 7 for wrong intervention, and 4 for wrong outcomes. Ultimately, 45 studies were included for data extraction. During full-text eligibility screening, each article was also reviewed by two reviewers.
Figure 2.
Flow diagram depicting the process of article identification, screening, and inclusion according to Preferred Reporting Items for Systematic Reviews and Meta-Analyses (PRISMA) guidelines. Both preclinical and clinical studies were included in the same article screening process.
3. Current Evidence for a Role of Modulating FAAH, MAGL, and DAGL Activity in Obesity-Related Outcomes
3.1. Animal Studies Involving Pharmacological Manipulation
We identified 5 animal studies that administered a pharmacological inhibitor of FAAH or DAGL and measured an obesity-related outcome (see Table 1).
Table 1.
Studies in animal models evaluating the impact of pharmacological manipulation of FAAH or DAGL enzymes on obesity-related outcomes.
Balsevich et al. (2018) investigated the role of FAAH in hypophagic responses to leptin [26]. Following a period of food deprivation, leptin administration induced expected reductions in body weight gain and food intake in saline-treated mice. Animals pre-treated with the FAAH inhibitor URB597 did not show these satiety responses following leptin treatment, suggesting that FAAH inhibition suppresses the effects of leptin on body weight and food intake. In another study, pharmacological inhibition of FAAH with PF-3845 had no effect on energy storage in rats [27]. Following exposure to a high-fat diet, PF-3845 and saline-treated animals showed similar decreases in body weight and food intake.
Stearoyl-CoA desaturase-1 (SCD1) is an enzyme involved in the synthesis of endogenous monounsaturated fatty acids (MUFAs). Due to its role in obesity, Liu et al. (2013) investigated functional interactions between SCD1 and ECS activity and found that MUFAs act as endogenous inhibitors of FAAH [28]. Under a high-fat diet, SCD1 knockout mice remained insulin-sensitive and glucose-tolerant compared to wildtype mice. When SCD1-deficient mice were treated with the FAAH inhibitor URB597, they became insulin resistant and showed increased sensitivity to glucose. Endogenous FAAH inhibition resulting from the SCD1-mediated production of MUFAs may thus contribute to the hyperinsulinemic phenotype in response to high-fat diets.
Two studies also investigated the use of DAGL inhibitors with obesity-related outcomes. Bisogno et al. (2013) found that the DAGLα inhibitor O-7460 significantly and dose-dependently reduced food intake in male mice under a high-fat diet [29]. The highest dose of O-7460 (12 mg/kg) was also associated with a small yet significant decrease in body weight. Palma-Chavez et al. (2019) used a shRNA DAGLα-inhibiting adenovirus to target tancytes of the hypothalamus and observed expression patterns of orexigenic (NPY) and anorexigenic (POMC) neuropeptides [30]. In fasting conditions, DAGLα inhibition was associated with reduced orexigenic and increased anorexigenic neuropeptides. Following glucose administration, DAGLα inhibition increased orexigenic and decreased anorexigenic neuropeptide expression. Control rats showed opposite responses in both conditions. Taken together, these findings indicate that DAGLα may regulate feeding behavior through the modulation of tancytic neuropeptides. DAGLα inhibition may reduce feeding through resulting decreases in 2-AG.
3.2. Animal Studies Involving Genetic Manipulation
We identified 11 preclinical studies involving the genetic manipulation of Faah, Mgll, or Dagla that reported obesity-related outcomes (see Table 2). All studies used C57BL/6 mouse models.
Table 2.
Studies in animal models evaluating the impact of genetic manipulation of Faah or Mgll on obesity-related outcomes.
The genetic deletion of Faah consistently produced obesity-related phenotypes across studies, as expected from resulting increases in AEA signaling. Greater body weight, fat mass, and triglyceride levels were observed in Faah knockout mice compared to wildtype under both standard and high-fat diets [31,32]. Faah-deficient mice also showed hepatic insulin resistance, which was associated with elevated liver triglyceride and diacylglycerol content [33]. The obesity phenotype found by Vaitheesvaran et al. (2012) in Faah-deficient mice was accompanied with greater total food intake under a regular diet [32]. In contrast, Touriño et al. (2010) found no effect of Faah deletion on food intake under either a standard or a high-fat diet [31]. However, Faah knockout mice showed greater reinforcement and motivational responses to food.
The FAAH C385A polymorphism is a common loss-of-function mutation in humans. The A-allele results in lower FAAH expression and has been associated with heightened obesity risk. Balsevich et al. (2018) generated a knock-in model of this variant and found impaired leptin sensitivity in A385A mice [26]. The expected reductions in food intake and body weight following leptin treatment seen in wildtype were absent in transgenic mice, suggesting a role of FAAH in leptin satiety responses.
In addition to hydrolyzing N-acylethanolamines (NAEs) such as AEA, FAAH terminates the signaling activity of N-acyl taurines (NATs). Grevengoed et al. (2019) engineered a Faah knock-in model that selectively impaired NAT catabolism without affecting NAE degradation [34]. The S268D substitution did not replicate the obesity phenotypes found in the other studies. Instead, transgenic mice showed an improved metabolic profile compared to wildtypes. These findings confirm that obesity phenotypes found in Faah-deficient models are the result of endocannabinoid accumulation rather than increased NATs. Elevated NAT levels may instead have beneficial effects on energy storage and metabolism, which remain to be investigated.
Five studies investigated the role of Mgll in energy storage and obesity-related measures. Overexpression of Mgll in forebrain neurons lowered endocannabinoid levels, causing expected reductions in weight gain and adiposity [35]. Interestingly, intestinal overexpression of Mgll produced the opposite phenotype, characterized by increased body fat mass and weight gain [36]. These contradicting findings may reflect tissue-specific functions of MAGL. Similarly, under an obesogenic diet, the genetic deletion of Mgll was associated with paradoxical improvements in metabolic function. Compared to wildtypes, Mgll-deficient mice experienced less weight gain, had lower plasma triglyceride levels, and lower hepatic triglyceride content [37,38]. Insulin sensitivity and glucose tolerance were also improved [38]. Under a low-fat diet, knockout mice had lower fat mass and body weight despite showing no significant differences in food intake [39]. Reduced triglyceride and cholesterol levels were also found in male Mgll knockout mice, under both low and high-fat diets. When males and females were considered together, this effect was only found in response to a high-fat diet. The potential sex-specific effects of Mgll function on energy storage were not investigated by the other studies, as they included only male mice.
Our search identified only one genetic manipulation study on Dagla and obesity-related measures. Powell et al. (2015) found that Dagla deletion improved metabolic function [40]. Compared to wildtype, knockout mice had reduced body weight, fat mass, total triglycerides and cholesterol. Food intake and fasting insulin levels were also reduced in Dagla-deficient mice.
3.3. Human Studies Involving Genetic Association
We identified 30 studies that included association between a FAAH or MGLL gene variant and any obesity-related outcome in a human sample (see Table 3). No studies were identified involving DAGLA or DAGLB gene variants. All 30 studies included at least one FAAH variant, with only 3 studies additionally examining variation in MGLL.
Table 3.
Human studies examining genetic association between FAAH and/or MGLL and obesity-related outcomes.
The majority of studies (26 out of 30) included one specific FAAH SNP, a missense mutation (C385A) associated with a change in amino acid sequence at position 129 from proline to threonine (Pro129Thr). This SNP was originally identified in 2002 and was found to be strongly associated with problematic substance use [41]. The Pro129Thr variant was found to have normal catalytic activity but an enhanced sensitivity to proteolytic degradation [41]. Subsequent functional characterization of the variant found that the mutant FAAH enzyme had less than half of the expression and activity of the wildtype enzyme [42].
Of the 26 studies included in the present review, 19 found a significant association between the C385A SNP and at least one obesity-related outcome [43,44,45,46,47,48,49,50,51,52,53,54,55,56,57,58,59,60,61]. Following up on their initial discovery of the C385A SNP, Sipe and colleagues were the first to identify a significant association between the A allele and increased likelihood of being overweight or obese in a sample of 1688 White adults and 614 Black adults (but not in 365 Asian adults) [57]. In support of these findings, Monteleone et al. (2008) found that the A allele was significantly more common in women who were overweight or obese compared to healthy weight controls (n = 299) [55]. Yagin et al. (2019) similarly found the A allele to be more common in women who were overweight or obese (n = 180) compared to health weight controls (n = 86) [60]. Thethi et al. (2020) recently reported another significant association between the A allele and obesity, though the association was no longer significant when controlling for age, race, sex, waist-to-hip ratio, and cholesterol [58]. Further support for an association between the C385A variant and increased risk of obesity comes from studies including continuous outcomes. For example, the A allele was associated with higher BMI, fat mass, and waist circumference in a sample of 70 participants with Type-II diabetes mellitus who were obese [50]. Yagin et al. (2019) also found a significant association between the A allele and higher BMI, waist circumference, neck circumference, waist-to-height ratio, and body fat mass [60], while Zhang et al. (2009) found an association between the A allele and higher BMI and triglyceride levels in a sample of 1644 participants from 261 pedigrees [61]. Further, Vazquez-Roque et al. (2011) found that A-allele carriers had a significantly greater maximum tolerated volume after a nutrient drink test, indicating lower satiety [59].
In contrast, multiple studies have failed to replicate the association between the A allele and obesity. Seven studies found no significant association between the SNP and any obesity-related outcomes [62,63,64,65,66,67,68]. A few studies actually found the reverse association—either a significant association between the wildtype (C/C) genotype and obesity [53,56] or an association of the wildtype (C/C) genotype with worse cardiometabolic outcomes, e.g., higher triglycerides and metabolic biomarkers [46]. Studies conducted by De Luis and colleagues failed to find any significant association between the C385A SNP and a wide range of obesity-related outcomes including anthropometric outcomes (BMI, body weight, waist circumference, etc.) and circulating lipids [44,45,46,47,48,49,51,52].
Interestingly, a number of studies have suggested that while the C385A SNP may not directly impact obesity-related outcomes at baseline, there may be an impact of the variant on changes in outcomes following either surgical or lifestyle interventions for obesity. Aberle et al. (2007) found that A-allele carriers had greater decreases in triglyceride and cholesterol levels after a 6-week low-fat diet intervention (n = 451 obese and dyslipidemic participants) [43]. Similarly, De Luis et al. (2011) found that A-allele carriers had greater improvement in a range of metabolic outcomes after 3 months of a hypocaloric dietary intervention (n = 122) [47], while De Luis et al. (2010) found greater weight loss in A-allele carriers at 9 and 12 months after biliopancreatic diversion surgery (n = 67) [51]. In contrast, three other studies by De Luis and colleagues found that the A-allele was associated with worse outcomes following either a low-fat or low-carbohydrate diet intervention for 3 months (n = 248) [52], and also following a 3-month enriched monounsaturated fat hypocaloric diet (n = 95) [44] and a 3-month enriched polyunsaturated fat hypocaloric diet (n = 99) [49]. Finally, Knoll et al. (2012) failed to show any association of the C385A variant and obesity-related outcomes after a 1-year diet and exercise intervention in a group of 453 overweight and obese children and adolescents [63].
In addition to examining associations between the FAAH C385A variant and obesity-related outcomes, four studies examined associations with other FAAH SNPs [53,56,61,64]. In a large sample of 5109 French Caucasian participants, Durand et al. (2008) failed to find an association between 10 FAAH SNPs and childhood obesity or Type-II diabetes mellitus, but did find a nominal association between 5 FAAH SNPs (rs6429600, rs324419, rs324418, rs2295633, and rs7520850) and Class III adult obesity [53]. Lieb et al. (2009) failed to find an association between 9 FAAH SNPs and obesity-related outcomes in a sample of 2415 participants from a longitudinal cohort [64]. Muller et al. (2010) found some additional evidence of association between FAAH gene variants and obesity—the G allele of rs2295632 was associated with early-onset obesity in 521 trios (children/adolescents and both biological parents), though this finding did not replicate in a second cohort of trios, and there was no association with obesity in adults (n = 8491 participants from a population-based study sample) [56]. Finally, Zhang et al. (2009) did not find an association between four FAAH SNPs (rs324418, rs1984490, rs2145408 and rs4141964) and any obesity-related traits [61].
Three studies used bioinformatic approaches to identify novel genetic variants in FAAH and MGLL genes associated with obesity or obesity-related traits [69,70,71]. Bhatia et al. (2010) used data from a large clinical trial cohort (n = 289) to identify rare variants in FAAH and MGLL associated with obesity, and found one significantly associated region of approximately 5 Kbp in the upstream regulatory region of each gene [69]. Harismendy et al. (2010) similarly used data from the same clinical trial cohort to identify one interval in the FAAH promoter and three intervals in MGLL (in the promoter, intron 2, and intron 3) that were all significantly associated with obesity [70]. Kuk et al. (2013) identified three potentially causal rare variants in MGLL associated with obesity, while also finding an interaction between two rare variants in FAAH that may increase the risk of obesity [71].
4. Discussion
The endocannabinoid system plays an important role in the regulation of hunger, satiety, and body weight. Obesity is associated with chronic over-activation of the ECS, with increased levels of circulating endocannabinoids. Thus, modulating the activity of ECS enzymes, thereby altering endocannabinoid signaling, is a biologically plausible strategy for treating obesity. Our review focused on obesity-related outcomes associated with manipulation of or variation in three key enzymes: FAAH, an enzyme responsible for degradation of many bioactive lipids, especially AEA; MAGL, another enzyme responsible for degradation, especially 2-AG; and DAGL, an enzyme involved in the synthesis of 2-AG. We identified 15 studies that involved pharmacological or genetic manipulation of at least one of these enzymes and assessment of at least one obesity-related outcome in an animal model, and 30 studies that examined a genetic association between variants in the genes encoding FAAH and MAGL and obesity in humans. Overall, we found strong evidence that modulating ECS enzyme activity can impact obesity-related outcomes, but the nature of the association is complex and likely dependent on numerous factors, such as species, age, sex, diet, and physical activity.
The preclinical studies reviewed found that either pharmacological inhibition or genetic deletion of FAAH produced obesogenic phenotypes, generally increased body weight, and/or worse metabolic outcomes. For example, Faah knockout mice had greater body weight, fat mass, and triglyceride levels compared to wildtype mice, under both a standard and high-fat diet [31,32]. It is important to note that there are many substrates of FAAH other than AEA (many of which do not act at CB receptors) and that the functions of FAAH substrates are incredibly diverse. Genetic deletion or pharmacological inhibition of FAAH produces a myriad of behavioural effects in animal models, including modulation of anxiety- and depressive-like behaviours, alterations in gastrointestinal function, decreases in pain response, decreases in inflammation, and modulation of drug-seeking behaviours and withdrawal [8]. As a result, FAAH inhibitors have been investigated in preclinical models of an incredibly wide range of pathological conditions, including pain (e.g., inflammatory, neuropathic, cancer-associated), neurological conditions (e.g., traumatic brain injury, epilepsy, movement-related disorders), gastrointestinal disorders, cardiovascular disorders, and psychiatric disorders (including substance use disorders) [21].
Of the human genetic association studies reviewed, most (26/30) focused on the rs324420 SNP of FAAH. Despite the initially compelling association between the A allele of this SNP and increased likelihood of being overweight and obese in a large sample of white and Black adults by Sipe and colleagues [57], which was replicated, at least in part, in three more recent studies [55,58,60], multiple studies have failed to find any association between rs324420 genotype and obesity [62,63,64,65,66,67,68]. In addition, two studies actually found a significant association between the homozygous major allele genotype (C/C) and obesity [53,56]. Of note, a handful of studies found that carriers of the A allele of rs324420 had greater improvements after either lifestyle (diet and/or exercise) intervention [43,47] or surgical intervention [51]. However, other studies failed to find greater improvement in A allele carriers [63] or found greater improvement associated with the major C/C genotype [44,49].
The effect of genetic manipulation of Mgll appears to be complex, and likely tissue-dependent. Preclinical studies found that overexpression of Mgll in forebrain neurons caused a reduction in weight gain and adiposity [35], yet intestinal overexpression of Mgll actually led to increased weight gain and fat mass [36]. The tissue-specific effects of Mgll deletion highlight the complexity of ECS control of energy intake and body weight. For example, MAGL is involved in the hydrolysis of triacylglycerols in adipose tissue [73]. Thus, future work should consider tissue-specific manipulation of MAGL on obesity-related outcomes, which may have important implications for therapeutic trials in humans.
Studies examining manipulation of DAGL were scarce. One study found that the DAGLα inhibitor O-7460 significantly decreased body weight in male mice [29], while another found that Dagla knockout mice had reduced body weight, fat mass, and total triglycerides compared to wildtype mice [40]. No human studies were identified that examined associations between DAGLA gene variants and obesity. This very preliminary evidence suggests that reducing biosynthesis of 2-AG could be one strategy to recapitulate the therapeutic effects of CB1 receptor antagonism, ideally without the serious psychiatric adverse effects as seen with rimonabant. Similarly, it could be worth exploring potential inhibitors of AEA biosynthesis. To date, there is no single enzyme purported to be the single “AEA synthase”, though N-acetylphosphatidylethanolamine-hydrolysing phospholipase D (NAPE-PLD) has been proposed as a candidate [8]. Interestingly, deletion of the gene encoding NAPE-PLD in mouse adipocytes induced an obese state characterized by glucose intolerance, adipose tissue inflammation, and altered lipid metabolism [74]. However, NAPE-PLD is involved in the biosynthesis of many other similar lipids, and NAPE-PLD genetic knockout does not consistently lead to a reduction in AEA [8].
While our review considered only candidate gene association studies in humans involving FAAH or MGLL, a brief note on genome-wide association studies (GWAS) of obesity is worthwhile. Small-scale candidate gene associations studies, such as some of the studies reviewed here, have been useful to identify specific monogenic forms of obesity, which are inherited in a Mendelian pattern and are typically rare, severe, with early onset [75]. Such approaches can also be used to identify common variants associated with polygenic (common) obesity. For example, candidate gene association approaches using larger samples were used to identify significant associations of variants in the CB1 receptor gene (CNR1) with obesity outcomes, which has been a reproducible association [76]. However, GWAS approaches using very large population samples are necessary to confirm the association of common variants contributing small effects to obesity [75]. Loos and Yeo (2021) extracted GWAS data from GWASCatalog, spanning from the first obesity GWAS in 2007 to 25 January 2021. A review of these data found no SNPs in FAAH, MGLL, or DAGLA/DAGLB that showed genome-wide significant association (p < 5 × 10⁻⁸) with obesity or related outcomes (also of note, no SNPs in CNR1 either) [75]. This suggests that variation in ECS genes is unlikely to make a major contribution to polygenic obesity, which is in line with the heterogeneity in results of candidate gene association studies (FAAH and obesity outcomes) we reviewed here.
Following up on the promising findings of preclinical animal studies of FAAH inhibition in multiple disease models, a number of human trials have been conducted or are ongoing to evaluate the potential of FAAH inhibitors across a range of indications [21]. For example, recently completed trials have found a positive signal for the FAAH inhibitor JNJ-42165279 in reducing anxiety symptoms in patients with social anxiety disorder [77] and the FAAH inhibitor PF-04457845 in reducing cannabis withdrawal in men with cannabis dependence [78]. A search of ClinicalTrials.gov identified a number of registered ongoing trials of FAAH inhibitors for substance use disorders, Tourette Syndrome, and pain. There have also been MAGL and dual FAAH/MAGL inhibitors developed to be evaluated in controlled trials. While our review has not provided clear evidence that FAAH or MAGL inhibitors would be useful for treating obesity, it will be worth noting whether there are any weight- or obesity-related effects observed in FAAH and/or MAGL inhibitor trials.
One final important consideration is the role of sex in modulating cannabinoid action. A wealth of preclinical data have established that sex significantly impacts the role of cannabinoids in multiple physiological processes, including pain, reward and addiction, and hunger and energy homeostasis [79,80]. For example, it has been demonstrated in rodent models that estradiol replacement in ovariectomized females tends to reduce energy intake in response to the CB1 receptor agonist WIN 55,212-2, while testosterone replacement in orchidectomized males tends to increase energy intake, which can be blocked by the CB1 receptor antagonist AM251 [80]. Unfortunately, the majority of the preclinical studies we reviewed conducted experiments in male animals only. Given that estrogens and testosterone may have divergent effects on energy intake (at least in rodents), future studies must consider sex as a biological variable in order to better understand how manipulation of the ECS may impact obesity differently in male and female bodies.
Taken together, the reviewed body of literature provides a mixed picture of whether FAAH, MAGL, or DAGL are likely to be druggable targets for obesity treatment. Studies in rodent models showed that reduction in FAAH activity leads to increased body weight and metabolic function, and while the human genetic association studies found consistent evidence of association between FAAH variants and obesity, the direction of effect was inconsistent. Thus, based on the evidence reviewed, FAAH inhibition is not likely a promising approach for obesity treatment. It will be prudent to monitor changes in body weight in ongoing trials of FAAH inhibitors for other indications. The role of MAGL modulation in obesity-related phenotypes appeared to be tissue dependent, with different effects depending on whether central or peripheral MAGL was targeted. Further research is needed to clarify this association. Based on a handful of animal studies, inhibition of DAGLα may be a promising strategy to treat obesity. This approach is in line with the higher levels of circulating endocannabinoids found in animals and humans with obesity. However, given the complex relationship between ECS activity and obesity, more evidence is needed to characterize the role of DAGL modulation in obesity. Human studies evaluating associations between DAGLA (and possibly also DAGLB) variants and obesity may provide some additional insight into whether modulating 2-AG synthesis impacts obesity-related outcomes.
Author Contributions
Conceptualization, J.M., X.M.M.Z., B.L.F.; methodology, J.M., X.M.M.Z., B.L.F.; data curation and article screening/review, J.M., X.M.M.Z., and Z.B.; writing—original draft preparation, J.M., X.M.M.Z., and Z.B.; writing—review and editing, all authors. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no direct external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Data sharing not applicable.
Acknowledgments
This article was supported by a Mitacs Accelerate Award to BLF in partnership with Canopy Growth Corporation.
Conflicts of Interest
Bernard Le Foll has obtained funding from Pfizer Inc. (GRAND Awards, including salary support) for investigator-initiated projects. Le Foll has obtained funding from Indivior for a clinical trial sponsored by Indivior. Le Foll has in-kind donations of cannabis products from Aurora Cannabis Enterprises Inc. and study medication donations from Pfizer Inc. (varenicline for smoking cessation) and Bioprojet Pharma. He was also provided a coil for a Transcranial magnetic stimulation (TMS) study from Brainsway. Le Foll has obtained industry funding from Canopy Growth Corporation (through research grants handled by the Centre for Addiction and Mental Health and the University of Toronto), Bioprojet Pharma, Alcohol Countermeasure Systems (ACS), and Alkermes. Lastly, Le Foll has received in kind donations of nabiximols from GW Pharmaceuticals for past studies funded by CIHR and NIH. He has participated in a session of a National Advisory Board Meeting (Emerging Trends BUP-XR) for Indivior Canada and has been consultant for Shinogi. He is supported by CAMH, a clinician-scientist award from the department of Family and Community Medicine of the University of Toronto and a Chair in Addiction Psychiatry from the department of Psychiatry of University of Toronto. Justin Matheson is currently supported by a Mitacs grant obtained by Le Foll in partnership with Canopy.
References
- NCD Risk Factor Collaboration (NCD-RisC). Trends in adult body-mass index in 200 countries from 1975 to 2014: A pooled analysis of 1698 population-based measurement studies with 19.2 million participants. Lancet 2016, 387, 1377–1396. [Google Scholar] [CrossRef] [Scilit]
- NCD Risk Factor Collaboration. Worldwide trends in body-mass index, underweight, overweight, and obesity from 1975 to 2016: A pooled analysis of 2416 population-based measurement studies in 128,9 million children, adolescents, and adults. Lancet 2017, 390, 2627–2642. [Google Scholar] [CrossRef] [Scilit]
- Guh, D.P.; Zhang, W.; Bansback, N.; Amarsi, Z.; Birmingham, C.L.; Anis, A.H. The incidence of co-morbidities related to obesity and overweight: A systematic review and meta-analysis. BMC Public Health 2009, 9, 88. [Google Scholar] [CrossRef] [Scilit]
- Spieker, E.A.; Pyzocha, N. Economic Impact of Obesity. Prim. Care 2016, 43, 83–95. [Google Scholar] [CrossRef] [Scilit]
- Richey, J.M.; Woolcott, O. Re-visiting the Endocannabinoid System and Its Therapeutic Potential in Obesity and Associated Diseases. Curr. Diab. Rep. 2017, 17, 99. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lu, H.C.; Mackie, K. An Introduction to the Endogenous Cannabinoid System. Biol. Psychiatry 2016, 79, 516–525. [Google Scholar] [CrossRef] [Scilit]
- Pamplona, F.A.; Takahashi, R.N. Psychopharmacology of the endocannabinoids: Far beyond anandamide. J. Psychopharmacol. 2012, 26, 7–22. [Google Scholar] [CrossRef] [Scilit]
- Gregus, A.M.; Buczynski, M.W. Druggable Targets in Endocannabinoid Signaling. Adv. Exp. Med. Biol. 2020, 1274, 177–201. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schulz, P.; Hryhorowicz, S.; Rychter, A.M.; Zawada, A.; Słomski, R.; Dobrowolska, A.; Krela-Kaźmierczak, I. What Role Does the Endocannabinoid System Play in the Pathogenesis of Obesity? Nutrients 2021, 13, 373. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rahmanian, M.; Lotfi Yaghin, N.; Alizadeh, M. Blood Level of 2-arachidonoyl glycerol (2-AG), Neuropeptide Y and Omentin and Their Correlation with Food Habits in Obese Women. Galen. Med. J. 2020, 9, e1721. [Google Scholar] [CrossRef] [Scilit]
- Côté, M.; Matias, I.; Lemieux, I.; Petrosino, S.; Alméras, N.; Després, J.P.; Di Marzo, V. Circulating endocannabinoid levels, abdominal adiposity and related cardiometabolic risk factors in obese men. Int. J. Obes. 2007, 31, 692–699. [Google Scholar] [CrossRef] [Scilit]
- Matias, I.; Gatta-Cherifi, B.; Tabarin, A.; Clark, S.; Leste-Lasserre, T.; Marsicano, G.; Piazza, P.V.; Cota, D. Endocannabinoids measurement in human saliva as potential biomarker of obesity. PLoS ONE 2012, 7, e42399. [Google Scholar] [CrossRef] [Scilit]
- Yagin, N.L.; Hajjarzadeh, S.; Aliasgharzadeh, S.; Aliasgari, F.; Mahdavi, R. The association of dietary patterns with endocannabinoids levels in overweight and obese women. Lipids Health Dis. 2020, 19, 161. [Google Scholar] [CrossRef] [Scilit]
- Azar, S.; Sherf-Dagan, S.; Nemirovski, A.; Webb, M.; Raziel, A.; Keidar, A.; Goitein, D.; Sakran, N.; Shibolet, O.; Tam, J.; et al. Circulating Endocannabinoids Are Reduced Following Bariatric Surgery and Associated with Improved Metabolic Homeostasis in Humans. Obes. Surg. 2019, 29, 268–276. [Google Scholar] [CrossRef] [Scilit]
- Murphy, T.; Le Foll, B. Targeting the Endocannabinoid CB1 Receptor to Treat Body Weight Disorders: A Preclinical and Clinical Review of the Therapeutic Potential of Past and Present CB1 Drugs. Biomolecules 2020, 10, 855. [Google Scholar] [CrossRef] [Scilit]
- Christopoulou, F.D.; Kiortsis, D.N. An overview of the metabolic effects of rimonabant in randomized controlled trials: Potential for other cannabinoid 1 receptor blockers in obesity. J. Clin. Pharm. Ther. 2011, 36, 10–18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Leite, C.E.; Mocelin, C.A.; Petersen, G.O.; Leal, M.B.; Thiesen, F.V. Rimonabant: An antagonist drug of the endocannabinoid system for the treatment of obesity. Pharmacol. Rep. 2009, 61, 217–224. [Google Scholar] [CrossRef] [Scilit]
- Christensen, R.; Kristensen, P.K.; Bartels, E.M.; Bliddal, H.; Astrup, A. Efficacy and safety of the weight-loss drug rimonabant: A meta-analysis of randomised trials. Lancet 2007, 370, 1706–1713. [Google Scholar] [CrossRef] [Scilit]
- Moreira, F.A.; Crippa, J.A. The psychiatric side-effects of rimonabant. Braz. J. Psychiatry 2009, 31, 145–153. [Google Scholar] [CrossRef] [Scilit]
- Le Foll, B.; Gorelick, D.A.; Goldberg, S.R. The future of endocannabinoid-oriented clinical research after CB1 antagonists. Psychopharmacology 2009, 205, 171–174. [Google Scholar] [CrossRef] [Scilit]
- Toczek, M.; Malinowska, B. Enhanced endocannabinoid tone as a potential target of pharmacotherapy. Life Sci. 2018, 204, 20–45. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Laleh, P.; Yaser, K.; Alireza, O. Oleoylethanolamide: A novel pharmaceutical agent in the management of obesity-an updated review. J. Cell Physiol. 2019, 234, 7893–7902. [Google Scholar] [CrossRef] [Scilit]
- Maccarrone, M.; Rossi, S.; Bari, M.; De Chiara, V.; Fezza, F.; Musella, A.; Gasperi, V.; Prosperetti, C.; Bernardi, G.; Finazzi-Agrò, A.; et al. Anandamide inhibits metabolism and physiological actions of 2-arachidonoylglycerol in the striatum. Nat. Neurosci. 2008, 11, 152–159. [Google Scholar] [CrossRef] [Scilit]
- Behl, T.; Chadha, S.; Sachdeva, M.; Sehgal, A.; Kumar, A.; Venkatachalam, T.; Hafeez, A.; Aleya, L.; Arora, S.; Batiha, G.E.S.; et al. Understanding the possible role of endocannabinoid system in obesity. Prostaglandins Other Lipid Mediat. 2021, 152, 106520. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Moura, E.D.M.; Dos Reis, S.A.; da Conceição, L.L.; Sediyama, C.; Pereira, S.S.; de Oliveira, L.L.; Gouveia Pelúzio, M.D.C.; Martinez, J.A.; Milagro, F.I. Diet-induced obesity in animal models: Points to consider and influence on metabolic markers. Diabetol. Metab. Syndr. 2021, 13, 32. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Balsevich, G.; Sticht, M.; Bowles, N.P.; Singh, A.; Lee, T.T.Y.; Li, Z.; Chelikani, P.K.; Lee, F.S.; Borgland, S.L.; Hillard, C.J.; et al. Role for fatty acid amide hydrolase (FAAH) in the leptin-mediated effects on feeding and energy balance. Proc. Natl. Acad. Sci. USA 2018, 115, 7605–7610. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cifani, C.; Avagliano, C.; Micioni Di Bonaventura, E.; Giusepponi, M.E.; De Caro, C.; Cristiano, C.; La Rana, G.; Botticelli, L.; Romano, A.; Calignano, A.; et al. Modulation of Pain Sensitivity by Chronic Consumption of Highly Palatable Food Followed by Abstinence: Emerging Role of Fatty Acid Amide Hydrolase. Front. Pharmacol. 2020, 11, 266. [Google Scholar] [CrossRef] [Scilit]
- Liu, J.; Cinar, R.; Xiong, K.; Godlewski, G.; Jourdan, T.; Lin, Y.; Ntambi, J.M.; Kunos, G. Monounsaturated fatty acids generated via stearoyl CoA desaturase-1 are endogenous inhibitors of fatty acid amide hydrolase. Proc. Natl. Acad. Sci. USA 2013, 110, 18832–18837. [Google Scholar] [CrossRef] [Scilit]
- Bisogno, T.; Mahadevan, A.; Coccurello, R.; Chang, J.W.; Allarà, M.; Chen, Y.; Giacovazzo, G.; Lichtman, A.; Cravatt, B.; Moles, A.; et al. A novel fluorophosphonate inhibitor of the biosynthesis of the endocannabinoid 2-arachidonoylglycerol with potential anti-obesity effects. Br. J. Pharmacol. 2013, 169, 784–793. [Google Scholar] [CrossRef] [Scilit]
- Palma-Chavez, A.; Konar-Nié, M.; Órdenes, P.; Maurelia, F.; Elizondo-Vega, R.; Oyarce, K.; López, S.; Rojas, J.; Steinberg, X.; García-Robles, M.A.; et al. Glucose Increase DAGLα Levels in Tanycytes and Its Inhibition Alters Orexigenic and Anorexigenic Neuropeptides Expression in Response to Glucose. Front. Endocrinol. 2019, 10, 647. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Touriño, C.; Oveisi, F.; Lockney, J.; Piomelli, D.; Maldonado, R. FAAH deficiency promotes energy storage and enhances the motivation for food. Int. J. Obes. 2010, 34, 557–568. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vaitheesvaran, B.; Yang, L.; Hartil, K.; Glaser, S.; Yazulla, S.; Bruce, J.E.; Kurland, I.J. Peripheral Effects of FAAH Deficiency on Fuel and Energy Homeostasis: Role of Dysregulated Lysine Acetylation. PLoS ONE 2012, 7, e33717. [Google Scholar] [CrossRef] [Scilit]
- Brown, W.H.; Gillum, M.P.; Lee, H.-Y.; Camporez, J.P.G.; Zhang, X.-M.; Jeong, J.K. Fatty acid amide hydrolase ablation promotes ectopic lipid storage and insulin resistance due to centrally mediated hypothyroidism. Proc. Natl. Acad. Sci. USA 2012, 109, 14966–14971. [Google Scholar] [CrossRef] [Scilit]
- Grevengoed, T.J.; Trammell, S.A.J.; McKinney, M.K.; Petersen, N.; Cardone, R.L.; Svenningsen, J.S.; Ogasawara, D.; Nexøe-Larsen, C.C.; Knop, F.K.; Schwartz, T.W.; et al. N-acyl taurines are endogenous lipid messengers that improve glucose homeostasis. Proc. Natl. Acad. Sci. USA 2019, 116, 24770–24778. [Google Scholar] [CrossRef] [Scilit]
- Jung, K.-M.; Clapper, J.R.; Fu, J.; D’Agostino, G.; Guijarro, A.; Thongkham, D.; Avanesian, A.; Astarita, G.; DiPatrizio, N.V.; Frontini, A.; et al. 2-Arachidonoylglycerol Signaling in Forebrain Regulates Systemic Energy Metabolism. Cell Metab. 2012, 15, 299–310. [Google Scholar] [CrossRef] [Scilit]
- Chon, S.-H.; Douglass, J.D.; Zhou, Y.X.; Malik, N.; Dixon, J.L.; Brinker, A.; Quadro, L.; Storch, J. Over-Expression of Monoacylglycerol Lipase (MGL) in Small Intestine Alters Endocannabinoid Levels and Whole Body Energy Balance, Resulting in Obesity. PLoS ONE 2012, 7, e43962. [Google Scholar] [CrossRef] [Scilit]
- Tardelli, M.; Bruschi, F.V.; Claudel, T.; Fuchs, C.D.; Auer, N.; Kunczer, V.; Stojakovic, T.; Scharnagl, H.; Habib, A.; Grabner, G.F.; et al. Lack of monoacylglycerol lipase prevents hepatic steatosis by favoring lipid storage in adipose tissue and intestinal malabsorption. J. Lipid Res. 2019, 60, 1284–1292. [Google Scholar] [CrossRef] [Scilit]
- Yoshida, K.; Kita, Y.; Tokuoka, S.M.; Hamano, F.; Yamazaki, M.; Sakimura, K.; Kano, M.; Shimizu, T. Monoacylglycerol lipase deficiency affects diet-induced obesity, fat absorption, and feeding behavior in CB1 cannabinoid receptor-deficient mice. FASEB J. 2019, 33, 2484–2497. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Douglass, J.D.; Zhou, Y.X.; Wu, A.; Zadrogra, J.A.; Gajda, A.M.; Lackey, A.I.; Lang, W.; Chevalier, K.M.; Sutton, S.W.; Zhang, S.P.; et al. Global deletion of MGL in mice delays lipid absorption and alters energy homeostasis and diet-induced obesity. J. Lipid Res. 2015, 56, 1153–1171. [Google Scholar] [CrossRef] [Scilit]
- Powell, D.R.; Gay, J.P.; Wilganowski, N.; Doree, D.; Savelieva, K.V.; Lanthorn, T.H.; Read, R.; Vogel, P.; Hansen, G.M.; Brommage, R.; et al. Diacylglycerol Lipase α Knockout Mice Demonstrate Metabolic and Behavioral Phenotypes Similar to Those of Cannabinoid Receptor 1 Knockout Mice. Front. Endocrinol. 2015, 6, 86. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sipe, J.C.; Chiang, K.; Gerber, A.L.; Beutler, E.; Cravatt, B.F. A missense mutation in human fatty acid amide hydrolase associated with problem drug use. Proc. Natl. Acad. Sci. USA 2002, 99, 8394–8399. [Google Scholar] [CrossRef] [Scilit]
- Chiang, K.P.; Gerber, A.L.; Sipe, J.C.; Cravatt, B.F. Reduced cellular expression and activity of the P129T mutant of human fatty acid amide hydrolase: Evidence for a link between defects in the endocannabinoid system and problem drug use. Hum. Mol. Genet. 2004, 13, 2113–2119. [Google Scholar] [CrossRef] [Scilit]
- Aberle, J.; Fedderwitz, I.; Klages, N.; George, E.; Beil, F.U. Genetic Variation in Two Proteins of the Endocannabinoid System and their Influence on Body Mass Index and Metabolism under Low Fat Diet. Horm. Metab. Res. 2007, 39, 395–397. [Google Scholar] [CrossRef] [Scilit]
- de Luis, D.; Aller, R.; Izaola, O.; Conde, R.; de la Fuente, B.; Sagrado, M.G. Genetic variation in the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) and their influence on weight loss and insulin resistance under a high monounsaturated fat hypocaloric diet. J. Diabetes Complicat. 2013, 27, 235–239. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Luis, D.A.; Aller, R.; Izaola, O.; Conde, R.; Sagrado, M.G.; Primo, D.; Castro, M.J. Relationship among metabolic syndrome, C358A polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) and insulin resistance. J. Diabetes Complicat. 2012, 26, 328–332. [Google Scholar] [CrossRef] [Scilit]
- de Luis, D.A.; González Sagrado, M.; Aller, R.; Izaola, O.; Conde, R. Relation of C358A polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) with obesity and insulin resistance. Nutr. Hosp. 2010, 25, 993–998. [Google Scholar] [PubMed]
- de Luis, D.A.; Gonzalez Sagrado, M.; Aller, R.; Izaola, O.; Conde, R. Effects of C358A missense polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase on weight loss after a hypocaloric diet. Metab. Clin. Exp. 2011, 60, 730–734. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Luis, D.A.; Gonzalez Sagrado, M.; Aller, R.; Izaola, O.; Conde, R.; Romero, E. C358A missense polymorphism of the endocannabinoid-degrading enzyme fatty acid amide hydrolase (FAAH) and visfatin levels in obese females. Int. J. Obes. 2010, 34, 511–515. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Luis, D.A.; Izaola, O.; Aller, R.; de La Fuente, B.; Pacheco, D. Effects of C358A polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) on weight loss, adipocytokines levels, and insulin resistance after a high polyunsaturated fat diet in obese patients. J. Endocrinol. Investig. 2013, 36, 965–969. [Google Scholar] [CrossRef] [Scilit]
- de Luis, D.A.; Sagrado, M.G.; Aller, R.; Izaola, O.; Conde, R.; Romero, E. C358A missense polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) and insulin resistance in patients with diabetes mellitus type 2. Diabetes Res. Clin. Pract. 2010, 88, 76–80. [Google Scholar] [CrossRef] [Scilit]
- de Luis, D.A.; Sagrado, M.G.; Pacheco, D.; Terroba, M.C.; Martin, T.; Cuellar, L.; Ventosa, M. Effects of C358A missense polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase on weight loss and cardiovascular risk factors 1 year after biliopancreatic diversion surgery. Surg. Obes. Relat. Dis. 2010, 6, 516–520. [Google Scholar] [CrossRef] [Scilit]
- de Luis, D.A.; Sagrado, M.G.; Aller, R.; Izaola, O.; Conde, R. Effects of C358A missense polymorphism of the degrading enzyme fatty acid amide hydrolase on weight loss, adipocytokines, and insulin resistance after 2 hypocaloric diets. Metab. Clin. Exp. 2010, 59, 1387–1392. [Google Scholar] [CrossRef] [Scilit]
- Durand, E.; Lecoeur, C.; Delplanque, J.; Benzinou, M.; Degraeve, F.; Boutin, P.; Marre, M.; Balkau, B.; Charpentier, G.; Froguel, P.; et al. Evaluating the Association of FAAH Common Gene Variation with Childhood, Adult Severe Obesity and Type 2 Diabetes in the French Population. Obes. Facts 2008, 1, 305–309. [Google Scholar] [CrossRef] [Scilit]
- Grolmusz, V.K.; Stenczer, B.; Fekete, T.; Szendei, G.; Patócs, A.; Rácz, K.; Reismann, P. Lack of Association between C385A Functional Polymorphism of the Fatty Acid Amide Hydrolase Gene and Polycystic Ovary Syndrome. Exp. Clin. Endocrinol. Diabetes 2013, 121, 338–342. [Google Scholar] [CrossRef] [Scilit]
- Monteleone, P.; Tortorella, A.; Martiadis, V.; Di Filippo, C.; Canestrelli, B.; Maj, M. The cDNA 385C to A missense polymorphism of the endocannabinoid degrading enzyme fatty acid amide hydrolase (FAAH) is associated with overweight/obesity but not with binge eating disorder in overweight/obese women. Psychoneuroendocrinology 2008, 33, 546–550. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Müller, T.D.; Brönner, G.; Wandolski, M.; Carrie, J.; Nguyen, T.T.; Greene, B.H.; Scherag, A.; Grallert, H.; Vogel, C.I.; Scherag, S.; et al. Mutation screen and association studies for the fatty acid amide hydrolase (FAAH) gene and early onset and adult obesity. BMC Med. Genet. 2010, 11, 2. [Google Scholar] [CrossRef] [Scilit]
- Sipe, J.C.; Waalen, J.; Gerber, A.; Beutler, E. Overweight and obesity associated with a missense polymorphism in fatty acid amide hydrolase (FAAH). Int. J. Obes. 2005, 29, 755–759. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Thethi, T.K.; Sigel, A.; Japa, S.; Katalenich, B.; Liu, S.; Nguyen, T.; Larrazolo, J.; Syu, S.; Carefoot, E.; McDuffie, R.; et al. Racial and sex differences in the polymorphisms of the endocannabinoid receptor genes in obesity. J. Diabetes Complicat. 2020, 34, 107682. [Google Scholar] [CrossRef] [Scilit]
- Vazquez-Roque, M.I.; Camilleri, M.; Vella, A.; Carlson, P.; Laugen, J.; Zinsmeister, A.R. Association of genetic variation in cannabinoid mechanisms and gastric motor functions and satiation in overweight and obesity. Neurogastroenterol. Motil. 2011, 23, 637-e257. [Google Scholar] [CrossRef] [Scilit]
- Yagin, N.L.; Aliasgari, F.; Aliasgharzadeh, S.; Mahdavi, R.; Akbarzadeh, M. The influence of the fatty acid amide hydrolase 385C>A single nucleotide polymorphisms on obesity susceptibility. Mol. Biol. Rep. 2019, 46, 5049–5055. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; Sonnenberg, G.E.; Baye, T.M.; Littrell, J.; Gunnell, J.; DeLaForest, A.; MacKinney, E.; Hillard, C.J.; Kissebah, A.H.; Olivier, M.; et al. Obesity-related dyslipidemia associated with FAAH, independent of insulin response, in multigenerational families of Northern European descent. Pharmacogenomics 2009, 10, 1929–1939. [Google Scholar] [CrossRef] [Scilit]
- Jensen, D.P.; Andreasen, C.H.; Andersen, M.K.; Hansen, L.; Eiberg, H.; Borch-Johnsen, K.; Jørgensen, T.; Hansen, T.; Pedersen, O. The functional Pro129Thr variant of the FAAH gene is not associated with various fat accumulation phenotypes in a population-based cohort of 5801 whites. J. Mol. Med. 2007, 85, 445–449. [Google Scholar] [CrossRef] [Scilit]
- Knoll, N.; Volckmar, A.L.; Pütter, C.; Scherag, A.; Kleber, M.; Hebebrand, J.; Hinney, A.; Reinehr, T. The Fatty Acid Amide Hydrolase (FAAH) Gene Variant rs324420 AA/AC is not Associated with Weight Loss in a 1-Year Lifestyle Intervention for Obese Children and Adolescents. Horm. Metab. Res. 2012, 44, 75–77. [Google Scholar] [CrossRef] [Scilit]
- Lieb, W.; Manning, A.K.; Florez, J.C.; Dupuis, J.; Cupples, L.A.; McAteer, J.B.; Vasan, R.S.; Hoffmann, U.; O’Donnell, C.J.; Meigs, J.B.; et al. Variants in the CNR1 and the FAAH Genes and Adiposity Traits in the Community. Obesity 2009, 17, 755–760. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mansouri, E.; Nobrega, J.N.; Hill, M.N.; Tyndale, R.F.; Lee, F.S.; Hendershot, C.S.; Best, L.M.; Di Ciano, P.; Balsevich, G.; Sloan, M.E.; et al. D3 dopamine receptors and a missense mutation of fatty acid amide hydrolase linked in mouse and men: Implication for addiction. Neuropsychopharmacology 2020, 45, 745–752. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Martins, C.J.D.M.; Genelhu, V.; Pimentel, M.M.G.; Celoria, B.M.J.; Mangia, R.F.; Aveta, T.; Silvestri, C.; Di Marzo, V.; Francischetti, E.A. Circulating Endocannabinoids and the Polymorphism 385C>A in Fatty Acid Amide Hydrolase (FAAH) Gene May Identify the Obesity Phenotype Related to Cardiometabolic Risk: A Study Conducted in a Brazilian Population of Complex Interethnic Admixture. PLoS ONE 2015, 10, e0142728. [Google Scholar] [CrossRef] [Scilit]
- Papazoglou, D.; Panagopoulos, I.; Papanas, N.; Gioka, T.; Papadopoulos, T.; Papathanasiou, P.; Kaitozis, O.; Papatheodorou, K.; Maltezos, E. The Fatty Acid Amide Hydrolase (FAAH) Pro129Thr Polymorphism is not Associated with Severe Obesity in Greek Subjects. Horm. Metab. Res. 2008, 40, 907–910. [Google Scholar] [CrossRef] [Scilit]
- Yagin, N.L.; Aliasgari, F.; Alizadeh, M.; Aliasgharzadeh, S.; Mahdavi, R. Comparison of endocannabinoids levels, FAAH gene polymorphisms, and appetite regulatory substances in women with and without binge eating disorder: A cross—Sectional study. Nutr. Res. 2020, 83, 86–93. [Google Scholar] [CrossRef] [Scilit]
- Bhatia, G.; Bansal, V.; Harismendy, O.; Schork, N.J.; Topol, E.J.; Frazer, K.; Bafna, V. A Covering Method for Detecting Genetic Associations between Rare Variants and Common Phenotypes. PLOS Comput. Biol. 2010, 6, e1000954. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Harismendy, O.; Bansal, V.; Bhatia, G.; Nakano, M.; Scott, M.; Wang, X.; Dib, C.; Turlotte, E.; Sipe, J.C.; Murray, S.S.; et al. Population sequencing of two endocannabinoid metabolic genes identifies rare and common regulatory variants associated with extreme obesity and metabolite level. Genome Biol. 2010, 11, R118. [Google Scholar] [CrossRef] [Scilit]
- Kuk, A.Y.C.; Li, X.; Xu, J. A fast collapsed data method for estimating haplotype frequencies from pooled genotype data with applications to the study of rare variants. Stat. Med. 2013, 32, 1343–1360. [Google Scholar] [CrossRef] [Scilit]
- Ning, T.; Zou, Y.; Yang, M.; Lu, Q.; Chen, M.; Liu, W.; Zhao, S.; Sun, Y.; Shi, J.; Ma, Q.; et al. Genetic interaction of DGAT2 and FAAH in the development of human obesity. Endocrine 2017, 56, 366–378. [Google Scholar] [CrossRef] [Scilit]
- Fredrikson, G.; Tornqvist, H.; Belfrage, P. Hormone-sensitive lipase and monoacylglycerol lipase are both required for complete degradation of adipocyte triacylglycerol. Biochim. Biophys. Acta 1986, 876, 288–293. [Google Scholar] [CrossRef] [Scilit]
- Geurts, L.; Everard, A.; Van Hul, M.; Essaghir, A.; Duparc, T.; Matamoros, S.; Plovier, H.; Castel, J.; Denis, R.G.; Bergiers, M. Adipose tissue NAPE-PLD controls fat mass development by altering the browning process and gut microbiota. Nat. Commun. 2015, 6, 6495. [Google Scholar] [CrossRef] [Scilit]
- Loos, R.J.F.; Yeo, G.S.H. The genetics of obesity: From discovery to biology. Nat. Rev. Genet. 2021, 1–14. [Google Scholar] [CrossRef] [Scilit]
- Benzinou, M.; Chèvre, J.C.; Ward, K.J.; Lecoeur, C.; Dina, C.; Lobbens, S.; Durand, E.; Delplanque, J.; Horber, F.F.; Heude, B.; et al. Endocannabinoid receptor 1 gene variations increase risk for obesity and modulate body mass index in European populations. Hum. Mol. Genet. 2008, 17, 1916–1921. [Google Scholar] [CrossRef] [Scilit]
- Schmidt, M.E.; Liebowitz, M.R.; Stein, M.B.; Grunfeld, J.; Van Hove, I.; Simmons, W.K.; Van Der Ark, P.; Palmer, J.A.; Saad, Z.S.; Pemberton, D.J.; et al. The effects of inhibition of fatty acid amide hydrolase (FAAH) by JNJ-42165279 in social anxiety disorder: A double-blind, randomized, placebo-controlled proof-of-concept study. Neuropsychopharmacology 2021, 46, 1004–1010. [Google Scholar] [CrossRef] [Scilit]
- D’Souza, D.C.; Cortes-Briones, J.; Creatura, G.; Bluez, G.; Thurnauer, H.; Deaso, E.; Bielen, K.; Surti, T.; Radhakrishnan, R.; Gupta, A.; et al. Efficacy and safety of a fatty acid amide hydrolase inhibitor (PF-04457845) in the treatment of cannabis withdrawal and dependence in men: A double-blind, placebo-controlled, parallel group, phase 2a single-site randomised controlled trial. Lancet Psychiatry 2019, 6, 35–45. [Google Scholar] [CrossRef] [Scilit]
- Cooper, Z.D.; Craft, R.M. Sex-Dependent Effects of Cannabis and Cannabinoids: A Translational Perspective. Neuropsychopharmacology 2018, 43, 34–51. [Google Scholar] [CrossRef] [Scilit]
- Wagner, E.J. Sex differences in cannabinoid-regulated biology: A focus on energy homeostasis. Front. Neuroendocrinol. 2016, 40, 101–109. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2021 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).