Article

Identification of a Major QTL and Development of a CAPS Marker Associated with Stem Blight Resistance in BC1 Populations Derived from Interspecific Crosses Between Asparagus officinalis L. and Asparagus kiusianus Makino


1
Graduate School of Bioresource and Bioenvironmental Sciences, Kyushu University, Motooka, Nishi-ku, Fukuoka 819-0395, Japan
2
Faculty of Agriculture, Kyushu University, Motooka, Nishi-ku, Fukuoka 819-0395, Japan
3
Institute of Tropical Agriculture, Kyushu University, Motooka, Nishi-ku, Fukuoka 819-0395, Japan
4
Faculty of Agriculture, Miyazaki University, Miyazaki 889-2192, Japan
5
Faculty of Agriculture, Kagawa University, Mikicho 761-0701, Kagawa, Japan
6
Graduate School of Life Science, Tohoku University, 2-1-1, Katahira, Aoba-ku, Sendai 980-8577, Japan
7
Kagawa Prefectural Agricultural Experiment Station, 1534-1 Ayagawa, Ayauta, Kagawa 761-2306, Japan
8
Institute of Vegetable and Floriculture Science, NARO (National Agriculture and Food Research Organization), Tsukuba 305-8519, Ibaraki, Japan
9
Kyushu Okinawa Agricultural Research Center, NARO (National Agriculture and Food Research Organization), 1823-1 Miimachi, Kurume 839-8503, Fukuoka, Japan
*
Authors to whom correspondence should be addressed.
Horticulturae 2026, 12(8), 953; https://doi.org/10.3390/horticulturae12080953
Submission received: 3 July 2026 / Revised: 26 July 2026 / Accepted: 28 July 2026 / Published: 2 August 2026
(This article belongs to the Section Biotic and Abiotic Stress)

Abstract

Stem blight, caused by Phomopsis asparagi, is the most serious disease affecting the cultivation of asparagus (Asparagus officinalis L.) in the warm regions of East and Southeast Asia, including Japan. Although Asparagus kiusianus, a wild species endemic to Japan, shows strong resistance to this disease and is cross-compatible with cultivated asparagus, the genetic basis of this resistance remains unclear. In this study, we used BC1 populations from interspecific crosses between A. officinalis and A. kiusianus to dissect stem blight resistance inheritance and identify markers suitable for marker-assisted selection. Disease severity was evaluated using P. asparagi inoculation, and RAD sequencing was used to construct a linkage map and perform QTL analysis. Segregation patterns suggested that resistance was controlled by major genes and polygenic factors which depended on the cross combination. A major QTL was detected on chromosome 1 and SNP_PRK showed a significant association (LOD > 3). A dCAPS marker derived from SNP_PRK was associated with resistance, with approximately 80% of individuals carrying the associated genotype showing resistance. CAPS marker PR1 distinguished the same genotype classes and produced results consistent with those obtained using PRK in the evaluated materials. PR1 may therefore facilitate resistant individual selection in breeding programs.

1. Introduction

Asparagus (garden asparagus: Asparagus officinalis L.) is a dioecious perennial herb belonging to the Asparagaceae family and is native to the Mediterranean region. It is utilized not only as a food crop but also as a source of bioactive compounds with potential health-promoting functions [1]. This plant can be harvested for over 10 years, with high economic value, and is widely cultivated across cold and temperate regions, including Europe, North and South America and northern China, as well as subtropical regions such as Mexico, southern China, and Southeast Asia. It is also extensively cultivated across Japan, from Hokkaido in the north to Kyushu in the south. The main diseases affecting asparagus are stem blight, spot disease, and brown spot disease, among which stem blight is the most significant constraint in open-field cultivation in the warm southwestern regions of Japan [2]. The primary control measure is rain-protected cultivation in plastic houses, but this is costly and involves harsh working conditions during the height of summer [3].
Stem blight is caused when the spores of Phomopsis asparagi, a fungus present on the soil surface, are splashed by rain and attach to young stems, leading to infection. As these stems elongate, the lesions expand, causing their aboveground parts to turn yellow and die. The pathogen overwinters as conidia and becomes a source of infection in the following year, making comprehensive control difficult. Therefore, there is strong demand for the development of stem blight-resistant varieties; however, no such varieties have been identified within A. officinalis [4]. Although relative species, such as A. densiflorus, A. virgatus, A. asparagoides, and A. macowanii, have shown strong resistance to the disease, they are all cross-incompatible with edible asparagus, which makes their practical use in breeding difficult [5].
Asparagus kiusianus is a relative species endemic to Japan, native to the coastal region from northern Kyushu to Yamaguchi Prefecture. It exhibits strong resistance to stem blight [6] and has been shown to be cross-compatible with A. officinalis [7]. Since interspecific hybrid plants combining A. kiusianus and asparagus have been reported to exhibit disease resistance similar to that of A. kiusianus alone [7], A. kiusianus serves as a key breeding resource for introducing stem blight resistance into asparagus. Takeuchi et al. [8] reported that the interspecific hybrids between A. officinalis and A. kiusianus had varying disease resistance depending on the cross combination. It is necessary to clarify the inheritance of disease resistance and to construct the genetic marker(s) for systematic breeding of disease-resistant cultivars.
In recent years, next-generation sequencing (NGS) technology has enabled development of numerous single-nucleotide polymorphic (SNP) markers in a single experiment through NGS-based genotyping by sequencing (GBS; [9]) and restriction site-associated DNA sequencing (RADseq; [10]). RADseq focuses on short DNA fragments adjacent to specific restriction enzyme recognition sites in order to identify genetic variations [10], and its application has been reported in many plant species, including eggplant [11], rice [12], soybean [13], and grape [14]. There have also been reports on SNP markers in asparagus, but the constructed linkage maps are sparse [15]. In addition, the focus on genetics in asparagus has been limited to sex [16], with no reports on disease resistance.
Based on the above background, the authors elucidated stem blight resistance trait inheritance in the hybrid progeny of A. officinalis and A. kiusianus, and attempted to develop SNP markers enabling efficient selection to achieve efficient breeding of asparagus varieties with strong resistance to stem blight disease.

2. Materials and Methods

2.1. Investigation of the Inheritance of Stem Blight Disease Resistance Character

2.1.1. Production of BC1 Individuals

One female accession, WC-9f, of asparagus ‘Welcome’, maintained at Kyushu University, and two interspecific male hybrids, OK007 and OK014, established by interspecific cross between asparagus strain AO0060F and A. kiusianus strain AK0501M at Tohoku University, were used. Interspecific back-crossings were conducted from April to July 2015 (Table 1). And fruit set at one month after pollination, harvested fruits and seeds, and seed germination were investigated.

2.1.2. Evaluation Time for Disease Severity Grades

The back-crossed (BC1) seedlings and 18 control asparagus plants obtained from the intraspecific crosses with ‘Welcome’, grown in plastic pots in an unheated greenhouse, were used for an inoculation test. Similar BC1 plants between asparagus ‘Welcome’ (WC2) and interspecific hybrid (WCK3) established at Kagawa Agricultural Experiment Station were also provided. Pathogen inoculation was performed from March to November 2016, following the method described by Iwato et al. [7] with slight modification. Specifically, a preserved strain of Phomopsis asparagi (P1) was cultured on potato dextrose agar (PDA) medium under black light blue (BLB) illumination at 25 °C. The strain was routinely stored at 4 °C and subcultured on PDA as needed; cultures were generally used after approximately 1–2 weeks of growth. Long-term serial subculturing was avoided, and the strain was renewed only when necessary for inoculum preparation. When reduced infectivity was observed, the strain was inoculated onto asparagus stems and subsequently re-isolated from infected tissues. The re-isolated strain was then used as a virulence-restored inoculum.
After pycnidium formation, a spore suspension was prepared at a concentration of 7.0 × 10⁶ spores/mL. The spore suspension was used as the treatment solution, and cotton wool soaked in the treatment solution was wrapped around the main stem of each plant that had resprouted after being cut back and had been growing for 2–3 weeks. The cotton was secured with vinyl tape to ensure proper inoculum contact.
Following inoculation, plants were maintained in a constant-temperature room at 25 °C and 80–90% relative humidity for 3 days. Then, the absorbent cotton and vinyl tape were removed, and the humidity was adjusted to 60–70%. From the day of inoculation until all of the control asparagus plants exhibited aboveground stem death, disease progression was assessed weekly.
Disease severity grade (DSG) was evaluated using the following disease scores in accordance with the previous report [7]:
0: No visible symptoms (healthy);
1: Small lesion formation (<1 cm);
2: Enlarged lesion covering less than half of the stem;
3: Large lesion covering more than half of the stem, or cladophyll abscission;
4: Complete or near-complete wilting of the aboveground part.
For subsequent analysis, disease resistance was categorized according to DSG values. Individuals with DSG scores of 0–2 were considered resistant, whereas those scoring 3–4 were classified as susceptible. Scores in the 0–2 range generally reflected limited lesion development that did not lead to severe damage or plant death, suggesting a degree of resistance. In contrast, scores of 3–4 were associated with severe disease symptoms, including extensive stem damage or complete wilting, and were therefore considered susceptible.
The progression of disease symptoms in BC1 plants was compared between the times when half of the control asparagus plants showed aboveground death and when all control plants did. The stage at which approximately 50% of the control plants exhibited aboveground death corresponded to an intermediate phase of disease development, at which symptoms were sufficiently expressed to allow clear discrimination among genotypes while avoiding saturation effects at later stages. Previous studies have shown that disease assessments conducted at intermediate stages of disease progression provide the highest resolution for distinguishing differences in host resistance [17,18].

2.1.3. Segregation of Stem Blight Disease Resistance in BC1 Progeny

Four BC1 populations, namely 65 seedlings from WC-9f × OK007, 116 from WC-9f × OK014, 32 from WC2 × WCK3 and 19 from OK011 × KAG WC No. 28, were provided for inoculation tests from March 2016 to November 2017. Eighteen asparagus seedlings were also used for the test as control, and inoculation methods followed the procedures outlined in Section 2.1.2. Disease progression was assessed when the percentage of aboveground stem mortality in control asparagus plants reached half.

2.2. Establishment of SNP Markers

2.2.1. Plant Materials and DNA Extraction

Genomic DNA was isolated from cladophyll tissues of one female asparagus plant (WC-9f), A. kiusianus, and two male interspecific hybrids (OK014 and OK007) using the potassium-based extraction method [19]. Approximately 30 mg of fresh, healthy cladophylls, free from visible damage or senescence, were collected from actively growing shoots for DNA extraction. The collected tissues were pulverized using a Multi-bead Shocker (Yasui Kikai, Osaka, Japan) equipped with three 1/8 size stainless beads (AS ONE, Osaka, Japan). The ground tissue was then combined with an extraction buffer composed of 100 mM Tris (pH 8), 50 mM EDTA, 500 mM NaCl and 1% SDS, along with 7 units of RNase (Qiagen, Hilden, Germany). The mixture was incubated at 65 °C for 90 min. Subsequently, one-third volume of 5 M potassium acetate was added to the lysate, which was then chilled on ice for 10 min. DNA was recovered by precipitation using an equal volume of isopropanol. After washing with 70% ethanol, the DNA was dissolved in 50 μL of TE buffer containing 10 mM Tris and 1 mM EDTA. The concentration of extracted DNA was standardized to approximately 20 ng/μL using the QuantiFluor™ dsDNA System (Promega, Madison, WI, USA) in conjunction with the Mx3000P Real-Time QPCR System (Agilent Technologies, Santa Clara, CA, USA).

2.2.2. Adjustment of Adapters

To construct the sequencing library, a dual-enzyme restriction digestion approach was applied, producing DNA fragments flanked by forward and reverse adapters. The forward adapters, each containing a unique barcode, were designed to match the KpnI restriction site overhang, while a universal reverse adapter was compatible with the MspI overhang. A set of 96 barcoded forward adapters with KpnI overhangs was generated using the Bar Coded Adapter Generator tool (http://www.deenabio.com/services/gbs-adapters: The website was last successfully accessed on 27 November 2017, but the link is currently inactive. The developer is Thomas Van Gurp.). The reverse adapter was structured as a Y-adapter to suppress amplification of MspI-MspI fragments. Adapter annealing was performed by heating to 95 °C for 1 min, followed by a gradual temperature decrease of 1 °C per cycle over 65 cycles. After ligation, adapter concentrations were measured using the same QuantiFluor™ system and QPCR setup, and normalized to 0.1 μM.

2.2.3. RAD Library Construction

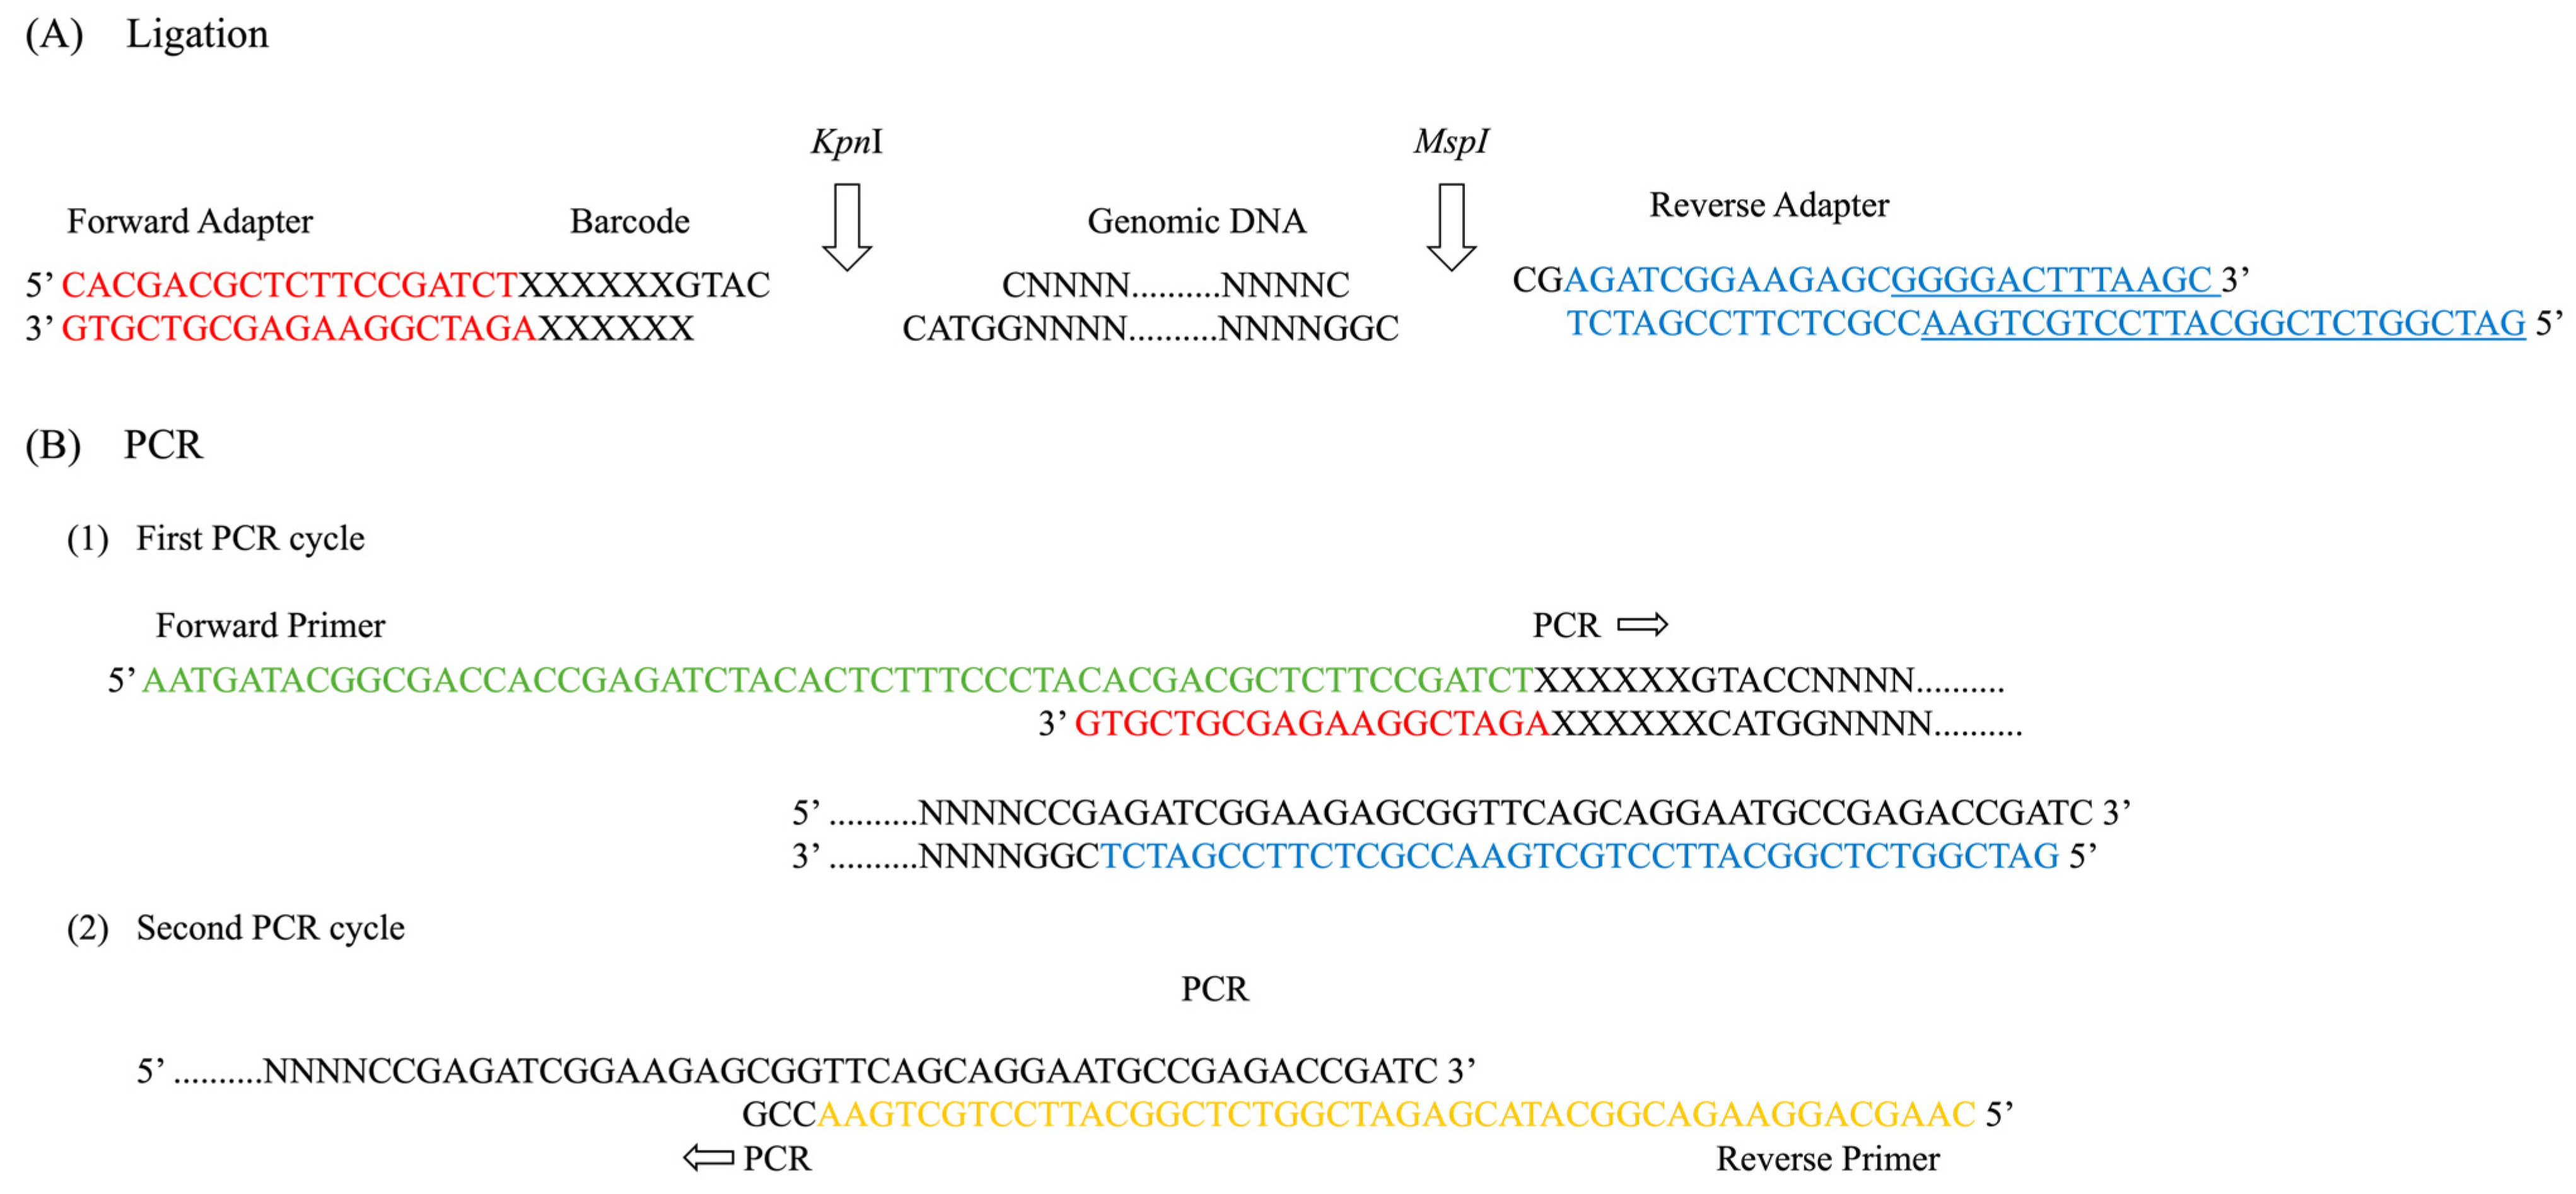
RADseq libraries were assembled following a modified version of the protocol by Poland et al. [20]. A total of 200 ng of genomic DNA was digested in a 20 μL reaction containing CutSmart Buffer (New England BioLabs, Ipswich, MA, USA) and 8 units each of KpnI-HF and MspI (New England BioLabs). The digestion was carried out at 37 °C for 2 h, followed by heat inactivation at 65 °C for 20 min. The resulting fragments were ligated to adapters compatible with Illumina flow cells (Figure 1A). Each sample received 0.1 pmol of forward adapter and 15 pmol of the common reverse adapter, along with CutSmart Buffer, 1 mM ATP (Thermo Fisher Scientific, San Jose, CA, USA), and 200 units of T4 DNA ligase (New England BioLabs). Ligation was performed at 22 °C for 2 h and terminated at 65 °C for 20 min. Ligated products were pooled and purified using the QIAquick PCR Purification Kit (Qiagen). Library amplification was conducted with an initial denaturation at 95 °C for 30 s, followed by 16 cycles of 95 °C (30 s), 62 °C (30 s), and 68 °C (30 s), and a final extension at 72 °C for 5 min (Figure 1B). A second purification step was performed post-PCR.

2.2.4. RAD Sequencing and SNP Identification

Sequencing was carried out on an Illumina MiSeq platform using the MiSeq Reagent Kit v3 (Illumina, San Diego, CA, USA), generating 86 bp reads from both ends. Base calling was performed using the TASSEL pipeline, which processes raw fluorescence signals into nucleotide sequences. These reads were aligned to the asparagus reference genome (https://www.ncbi.nlm.nih.gov/genome/?term=asparagus: accessed on 27 November 2017) using the Burrows-Wheeler Aligner (BWA). SNP identification and base quality recalibration were executed using a custom Java script available from the TASSEL software suite (http://www.maizegenetics.net/tassel: accessed on 27 November 2017).

2.2.5. Linkage Map Construction and QTL Analysis

Based on the RAD sequencing analysis results, linkage map construction and QTL analysis were performed using the genetic linkage analysis software JoinMap 4.0 (https://www.kyazma.nl/index.php/JoinMap/: accessed on 27 November 2017) and MapQTL 6 (https://www.kyazma.nl/index.php/MapQTL/: accessed on 27 November 2017). A linkage map was constructed by grouping with LOD scores ranging from 3.0 to 8.0, and by the application of the Maximum Likelihood (ML) method.

2.2.6. Development of dCAPS (PRK) and CAPS (PR1) Markers for Stem Blight Resistance

The SNP_PRK identified through the linkage map and QTL analysis as being associated with resistance was dCAPS-modified to facilitate the detection of polymorphisms. The dCAPS marker, PRK (where PR represents Phomopsis resistance and K represents kiusianus), was designed using the primer pair PRK_Fw (5′-CAAGAATCTCTCCTTCACTATCAACCACAG-3′, with an artificially introduced mismatch base G at the 3′ end) and PRK_Rv (5′-GCGTGTTTGATGCTAAGATTATGCCTTTGA-3′), with BsmAI (recognition sequence: GTCTC) as the restriction enzyme. Screening was performed on 66 individuals in the BC1 population using the PRK marker. The association between PRK genotype and resistance phenotype, classified as DSG 0–2 (resistant) and DSG 3–4 (susceptible), was evaluated using a chi-square test of independence, and the strength of the association was quantified using Cramér’s V. To evaluate the robustness of this cutoff, all four possible contiguous binary divisions of the five-level DSG scale were compared. In addition, exploratory one-dimensional k-means clustering (k = 2) was performed using the individual DSG scores independently of PRK genotype. The optimal two-cluster partition was defined as the partition with the minimum total within-cluster sum of squares (WCSS). However, in some asparagus individuals, the banding pattern was occasionally unstable and could not be reliably scored. Therefore, a new CAPS marker, PR1, was developed based on sequences flanking the PRK region.
The PR1 marker was designed using the primer pair PR1_Fw (5′-CCTATTCGGCCACCAGGACC-3′) and PR1_Rv (5′-CAGCTGTCGCTTGTTGGTTGTC-3′). PCR amplification was performed in a total volume of 25 µL containing 100 ng template DNA, 0.5 µM of each primer, 0.2 mM of each dNTP, 2.5 µL 10× PCR Ex Taq buffer, and 0.5 Unit Ex Taq polymerase. Amplification was carried out with one cycle of 2 min at 94 °C, followed by 35 cycles of 30 s at 94 °C, 30 s at 55 °C, and 1 min at 72 °C, and finally one cycle of 10 min at 72 °C. The amplified products were digested in a total volume of 20 µL containing 10.0 µL PCR product, 2.0 µL 10× M buffer, 2.0 µL BSA, and 10 Unit XbaI at 37 °C for 2 h, followed by enzyme inactivation at 65 °C for 15 min. For electrophoresis, 5.0 µL of the digested product was mixed with 1.0 µL of 6× Loading Dye and separated on a 1% agarose gel.

3. Results

3.1. Investigation of Stem Blight Disease Resistance Characteristic Inheritance

3.1.1. Production of BC1 Individuals

The results of the crossing experiments are summarized in Table 1. The fruit set rates were 49.0% and 68.9% in WC-9f × OK007 and WC-9f × OK014, respectively, and the fruit harvest rate averaged 54.2%. Commercial asparagus cultivars can, typically, produce up to six seeds per fruit, and the average number of seeds per fruit reached 2.3 to 3.1 in the interspecific back-crosses. Seed germination rates were relatively high, ranging from 74.2 to 84.3%.

3.1.2. Evaluation Time for Disease Severity Grades

Comparing half of and all of the control asparagus plants, they showed aboveground death at 4 to 8 and 7 to 11 weeks after inoculation, respectively. When half of the control plants had their aboveground stems die off, the remaining half were all DSG 3.
In all BC1 populations, individual variation was observed in both disease onset and symptom progression. Specifically, regarding the timing of symptom onset, individuals ranged from showing symptoms as early as one week after inoculation to showing no symptoms even after seven weeks. The disease progression rate also varied among individuals, with some showing a gradual progression from DSG 1 to DSG 4, the disease severity increasing by one grade each week, and the aboveground stems dying after 4 weeks. Others showed no symptoms one week after inoculation but developed DSG3 after 2 weeks.
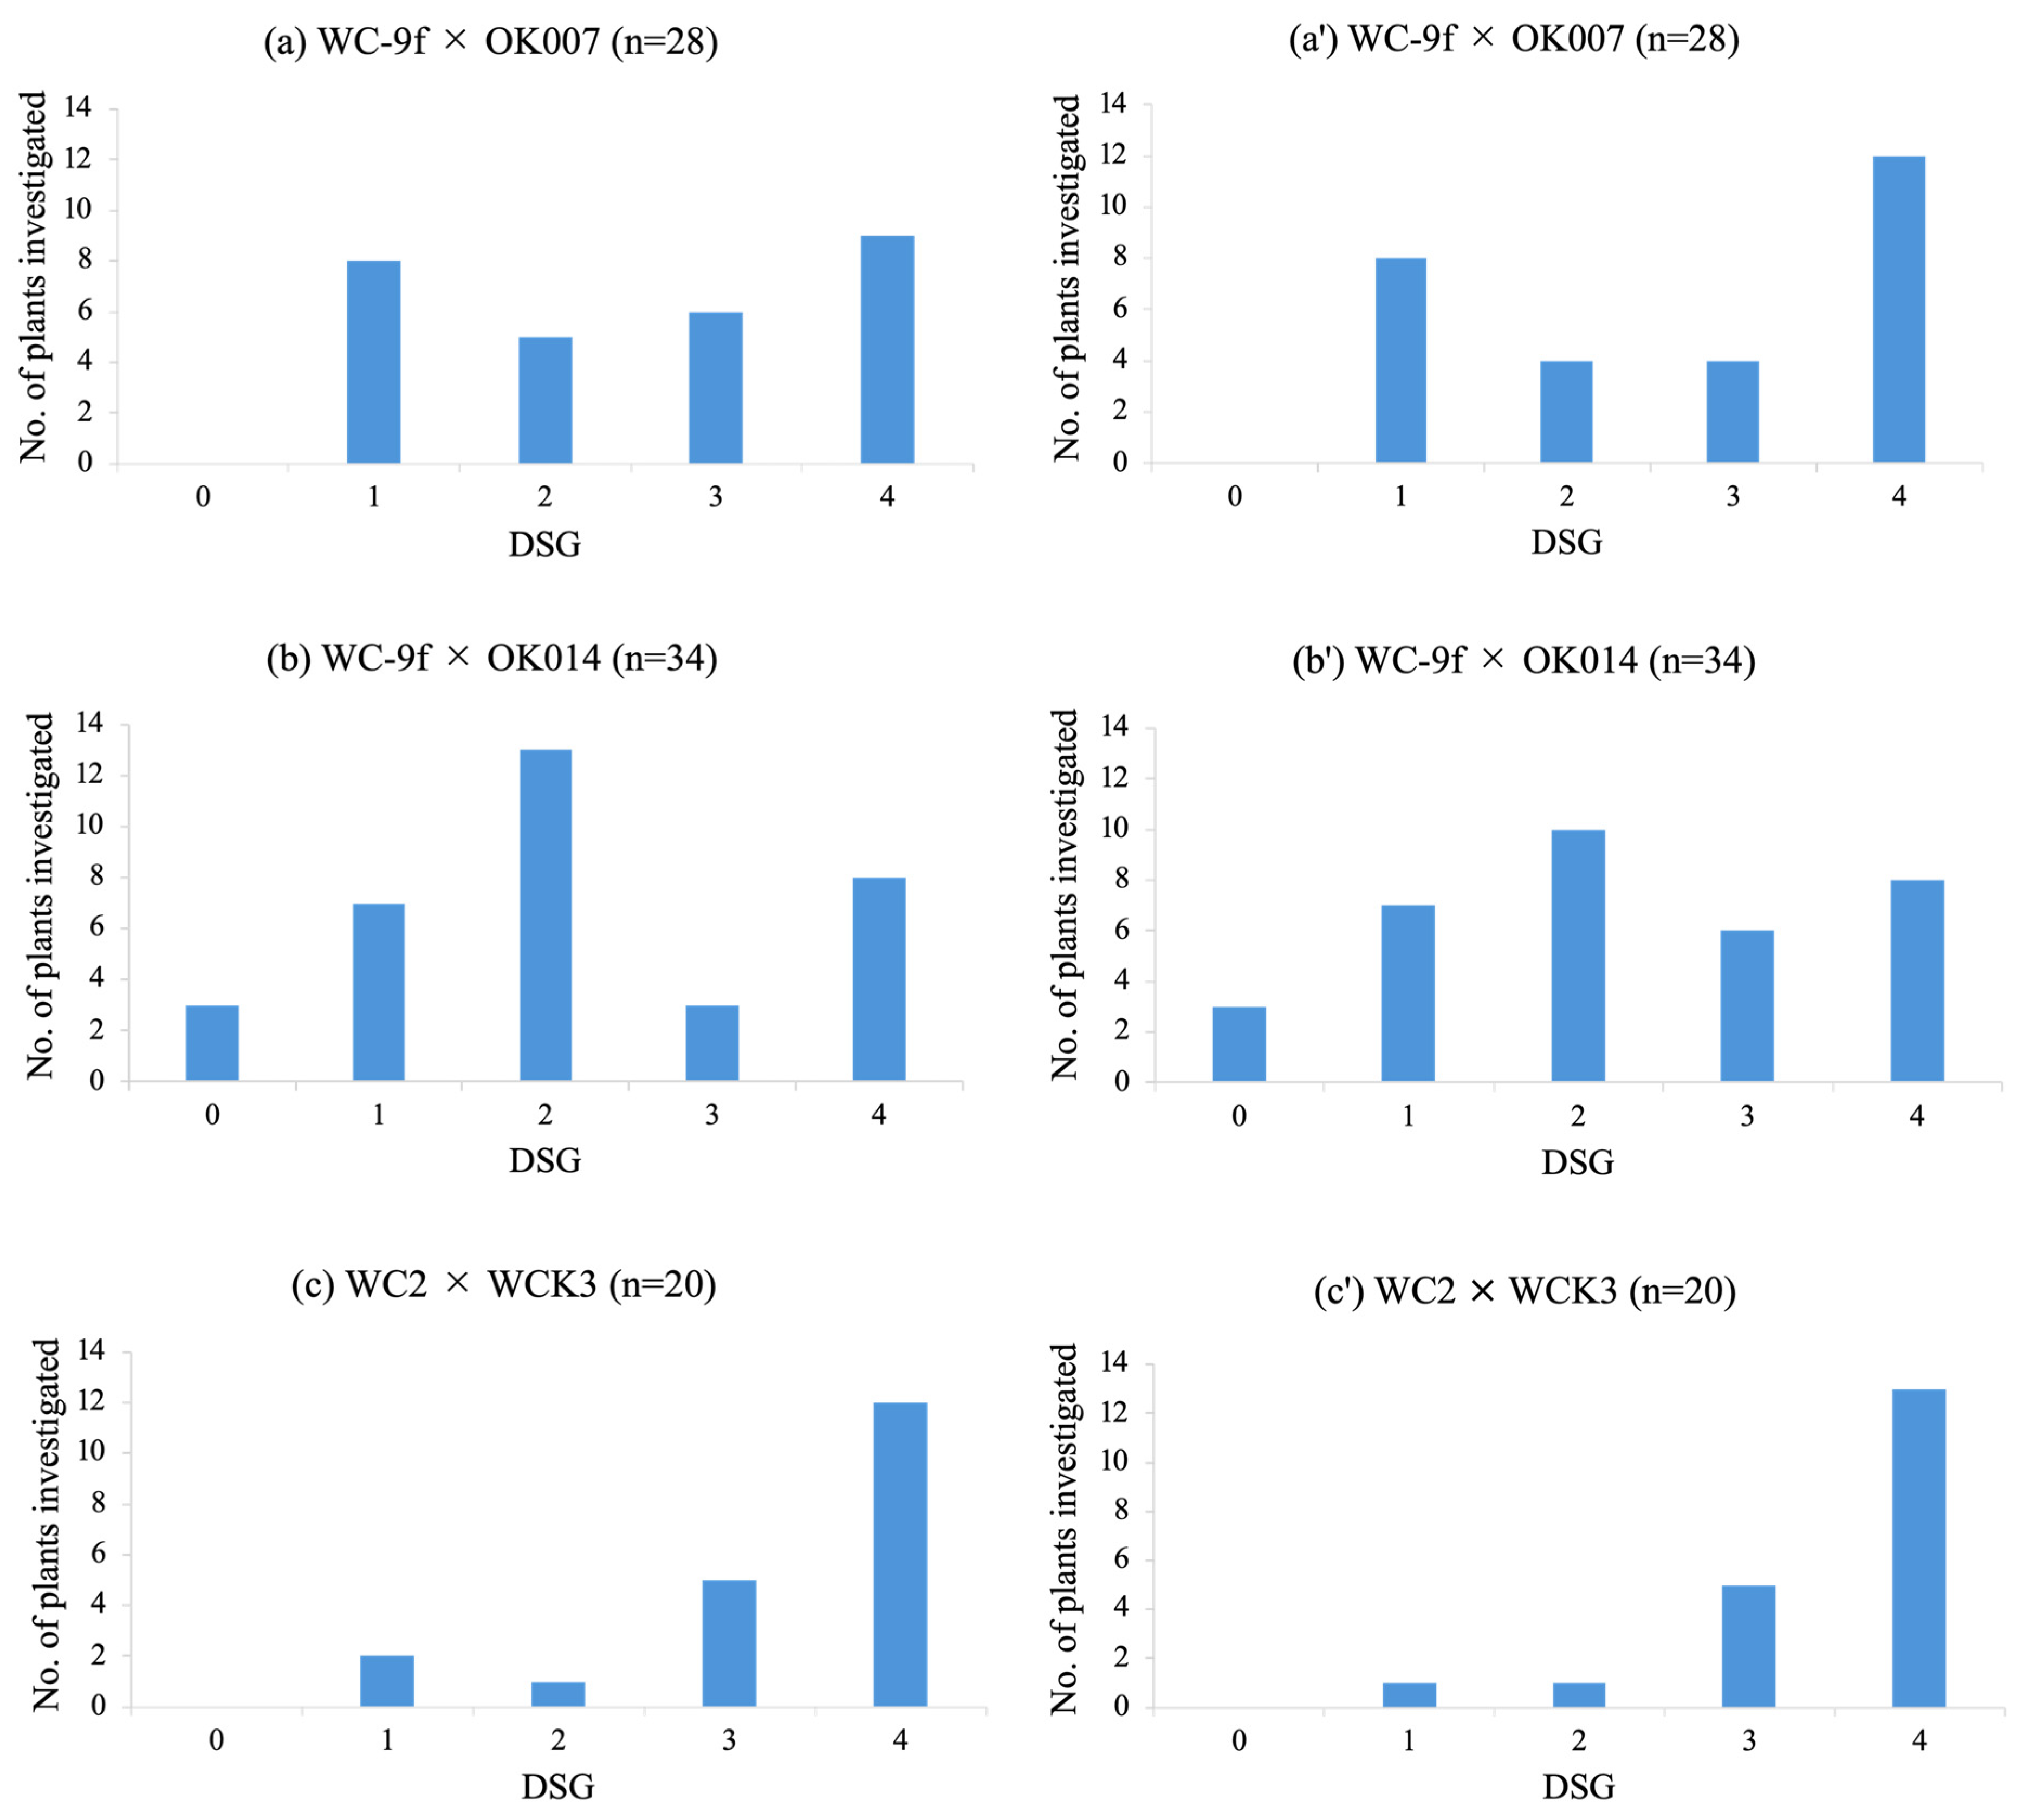
Figure 2 shows the frequency distributions of individuals with their DSGs from three crosses (WC-9f × OK007, WC-9f × OK014, and WC2 × WCK3) at different evaluation time points, with the patterns of individuals’ disease severity grades representing a similar tendency between the two evaluation time points in each cross. Based on the results, the evaluation time point for early diagnosis was defined as when half of the control asparagus plants showed aboveground stem death.

3.1.3. Segregation of Stem Blight Disease Resistance in BC1 Progeny

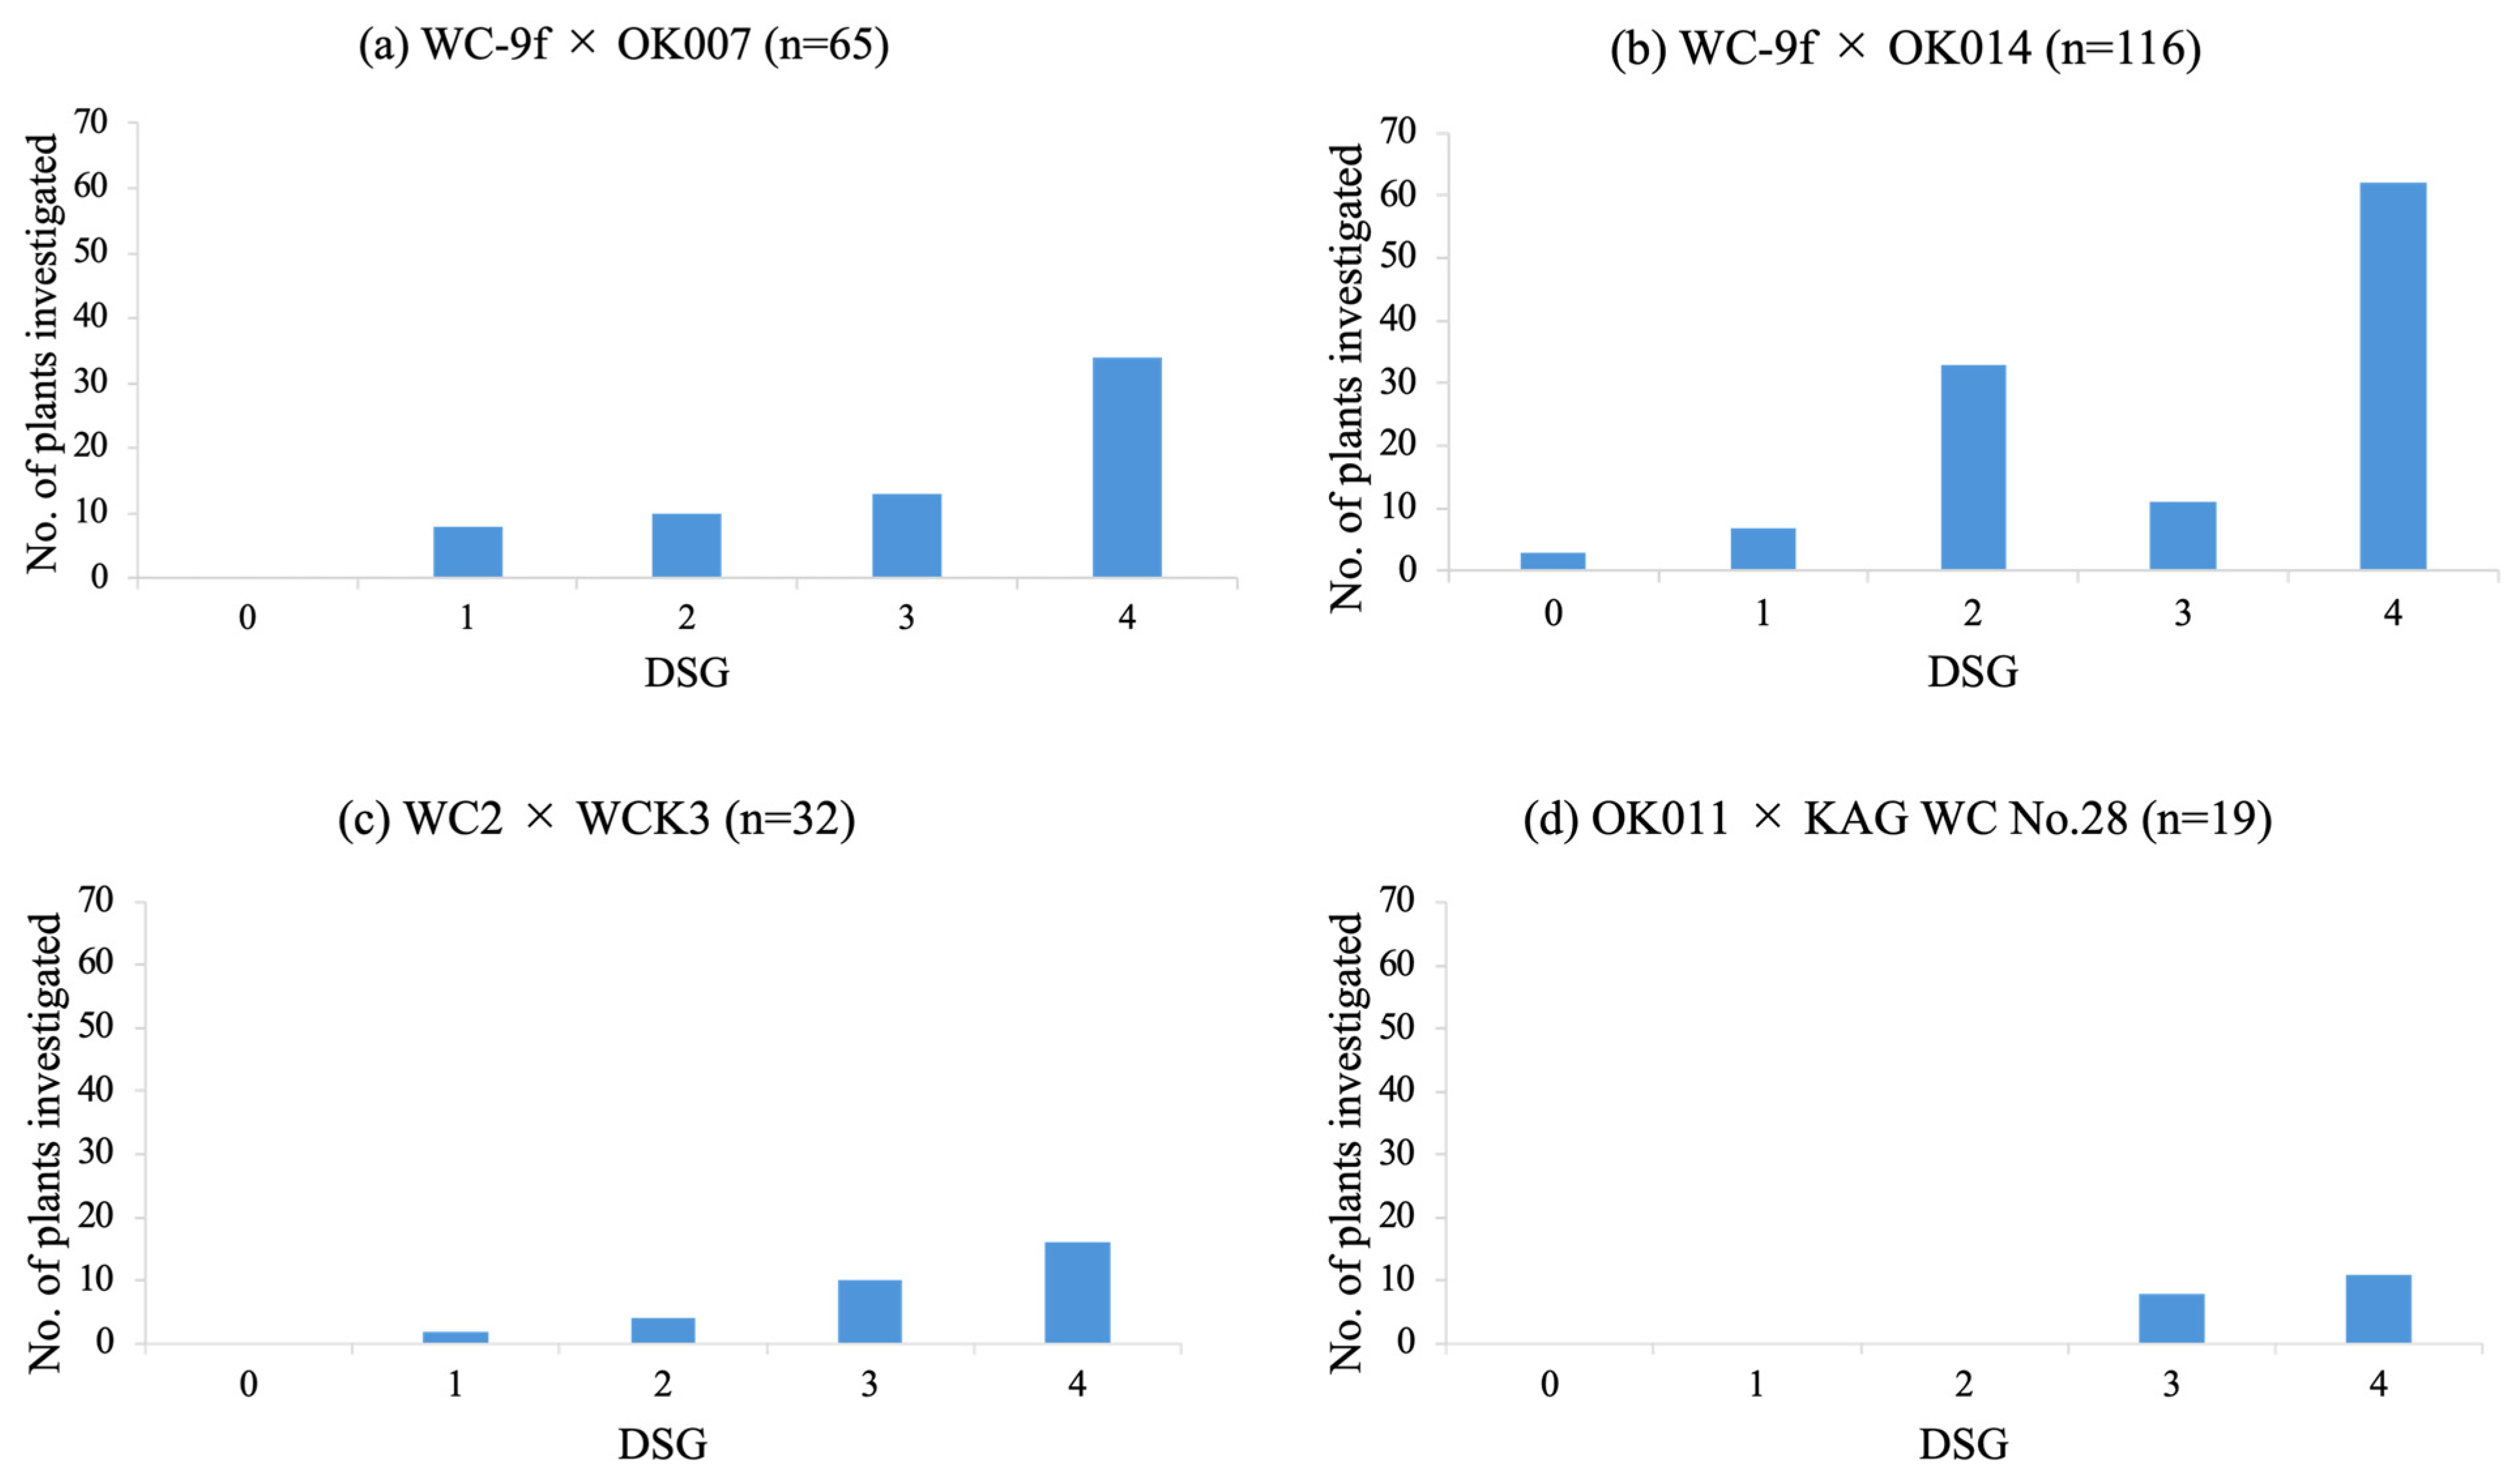
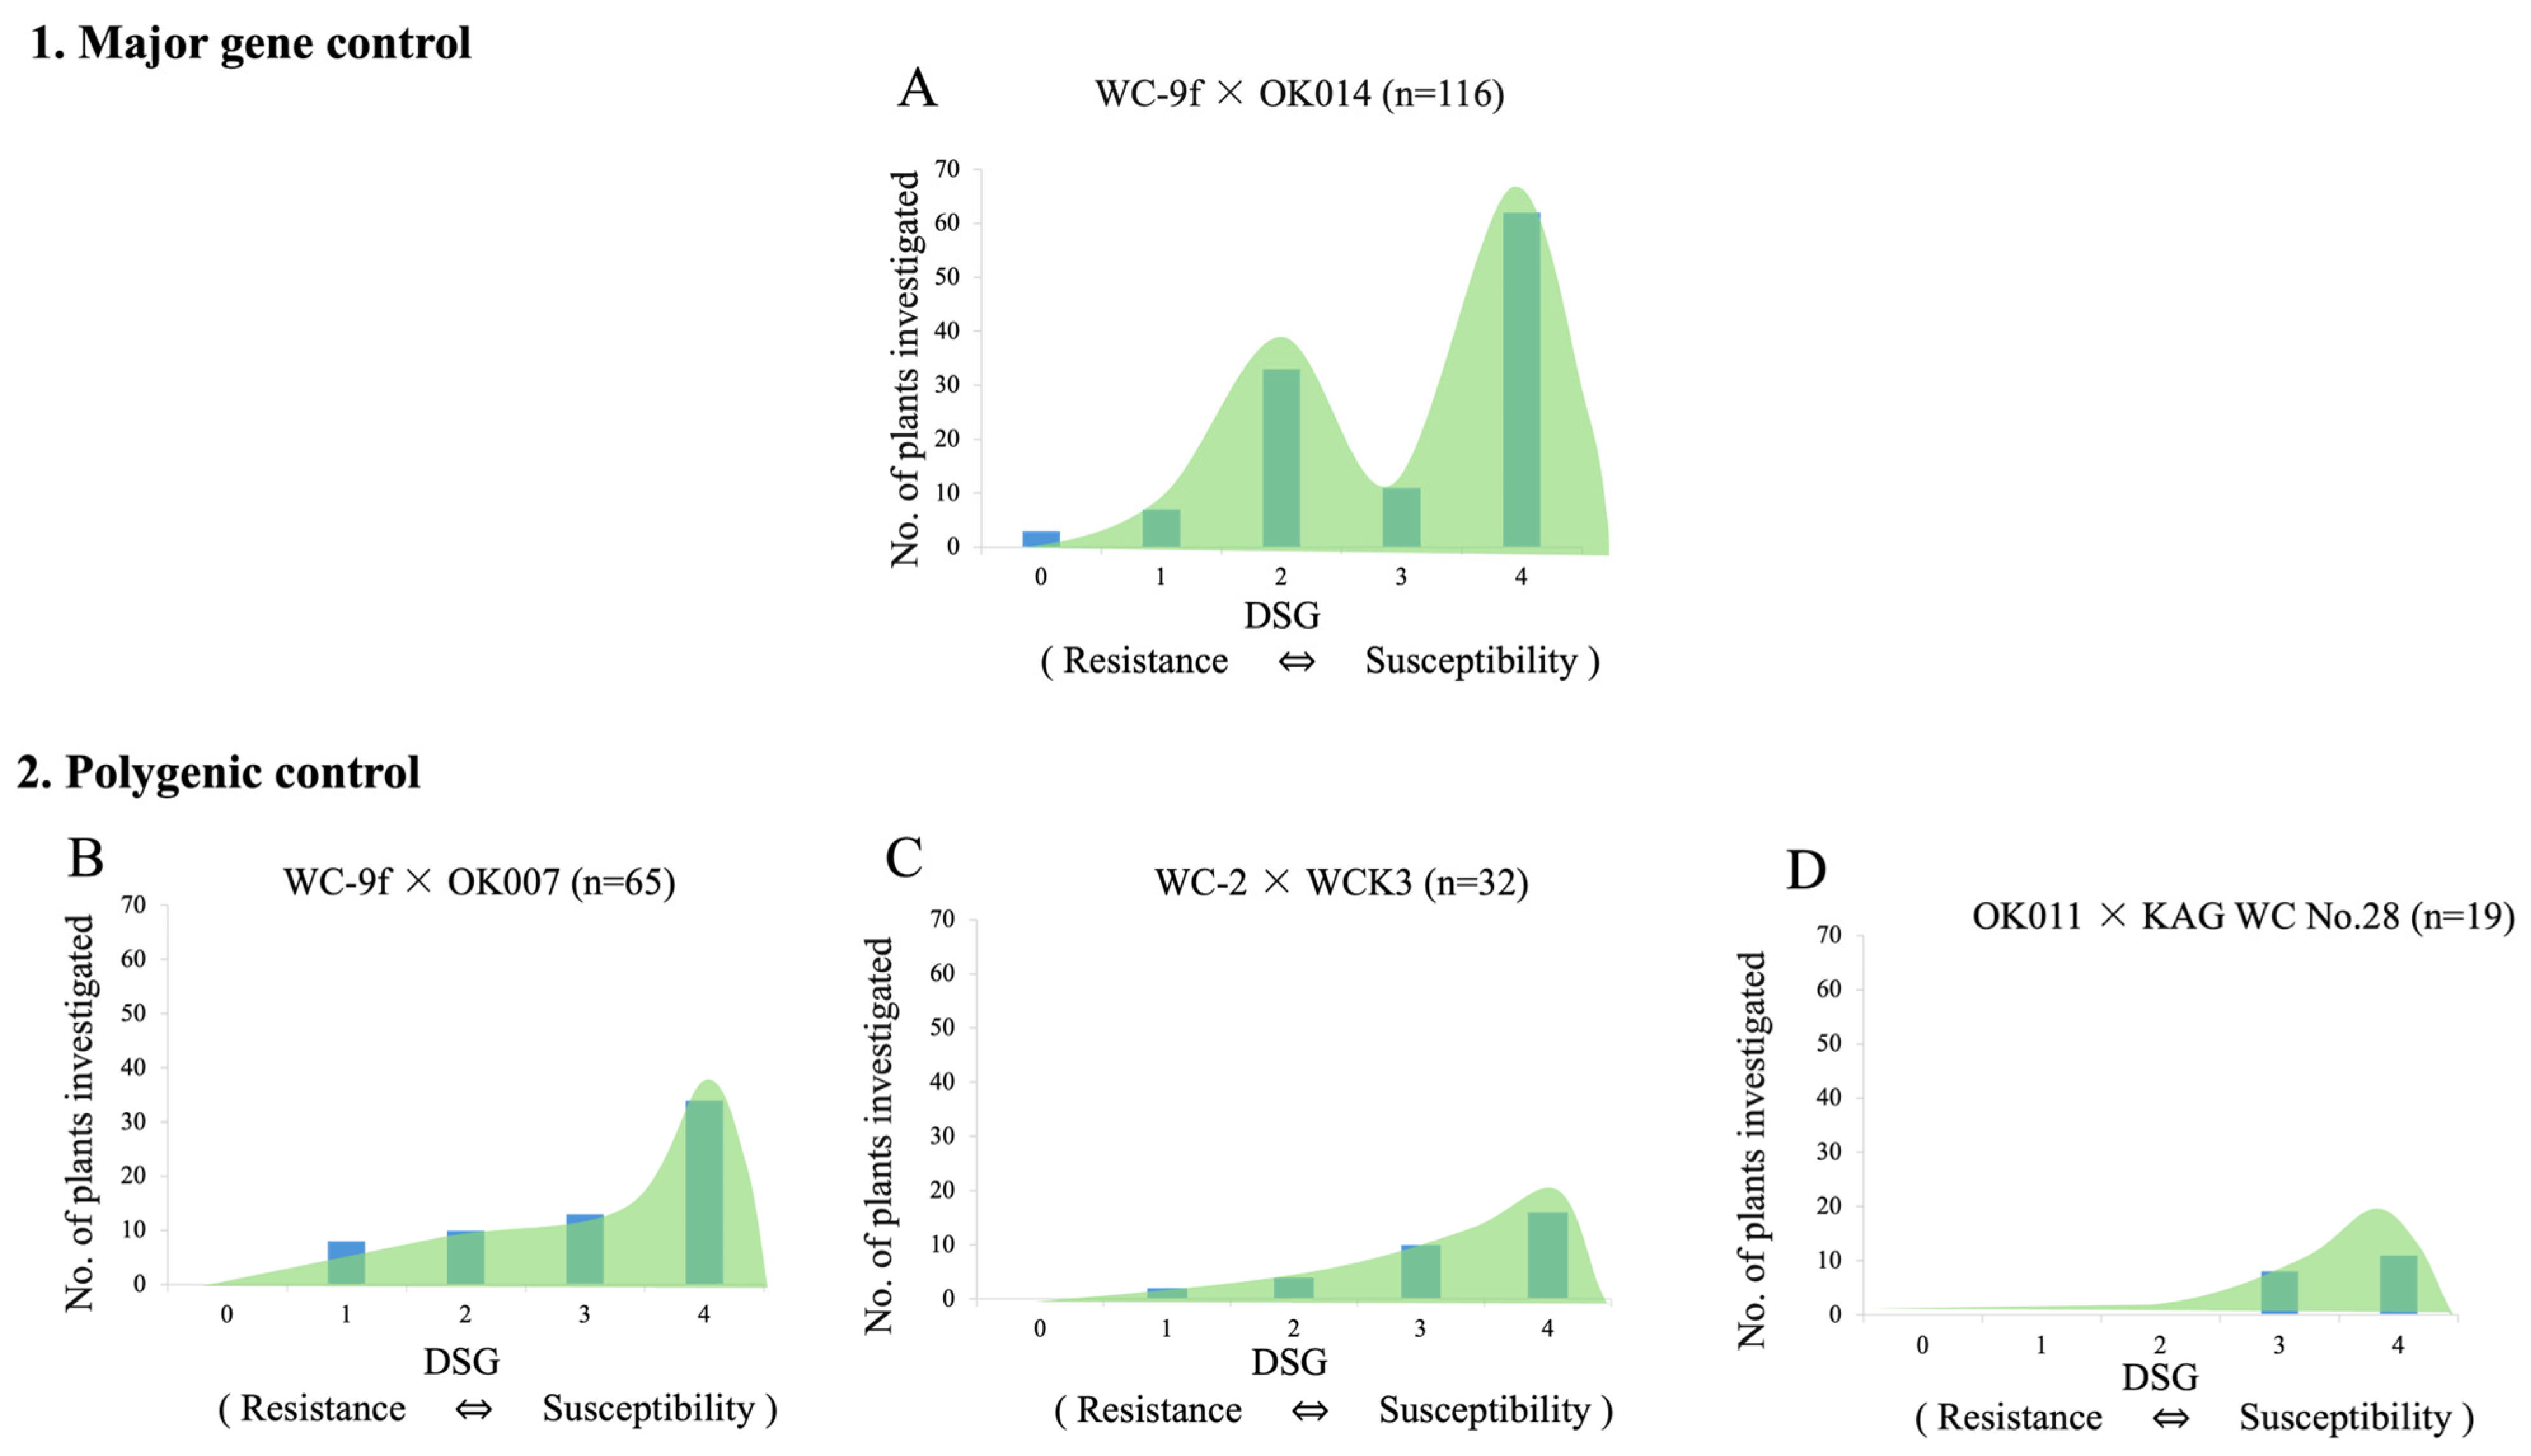
Figure 3 shows the segregation of the number of individuals in each disease severity grade category, with the patterns differing among cross combinations. In WC-9f × OK014, a bimodal distribution with peaks at DSG 2 and DSG 4 was observed, suggesting separation into a relatively resistant and a clearly susceptible group. In contrast, in WC-9f × OK007, WC2 × WCK3, and OK011 × KAG WC No. 28, the distributions were more continuous and shifted toward higher disease severity grade values; the largest number of lines were classified as DSG 4, whereas only a small number fell into the lower disease severity grade classes.
Segregation of stem blight resistance in the BC1 progeny was dependent on the cross combination, and the WC-9f × OK014 segregation pattern was markedly different from those of the other crosses.

3.2. Establishment of SNP Markers

3.2.1. Identification of SNPs and Genotyping

Since the involvement of a major gene was anticipated based on the segregation of resistant and susceptible individuals in the WC-9f × OK014 population, those with a DSG of 0–2 and 3–4 were provisionally classified as “resistant (Rr)” and “susceptible (rr)”, respectively.
A total of 3393 SNPs were detected (hk × hk: 525; nn × np: 2298; lm × ll: 570) between WC-9f and OK014. Genotyping of the parental individuals of OK014, AO0060F and AK0501M revealed that the p of 2103 nn × np SNPs was derived from A. kiusianus, and they were utilized for mapping. As OK007 was also derived from the same cross, AO0060F × AK0501M, SNPs showing the same genotype between OK014 and OK007 were selected for the integrated analysis. As a result, a total of 2624 SNPs were identified (hk × hk: 404; nn × np: 1748; lm × ll: 472) between WC-9f and “OK007 + OK014”, and the p of 1581 nn × np markers was derived from A. kiusianus. In addition to these SNPs, the previously mentioned resistant genotype and 21 RNA-seq-derived markers [6,21] were incorporated into the mapping analysis.

3.2.2. Integration of Populations and Construction of the Linkage Map

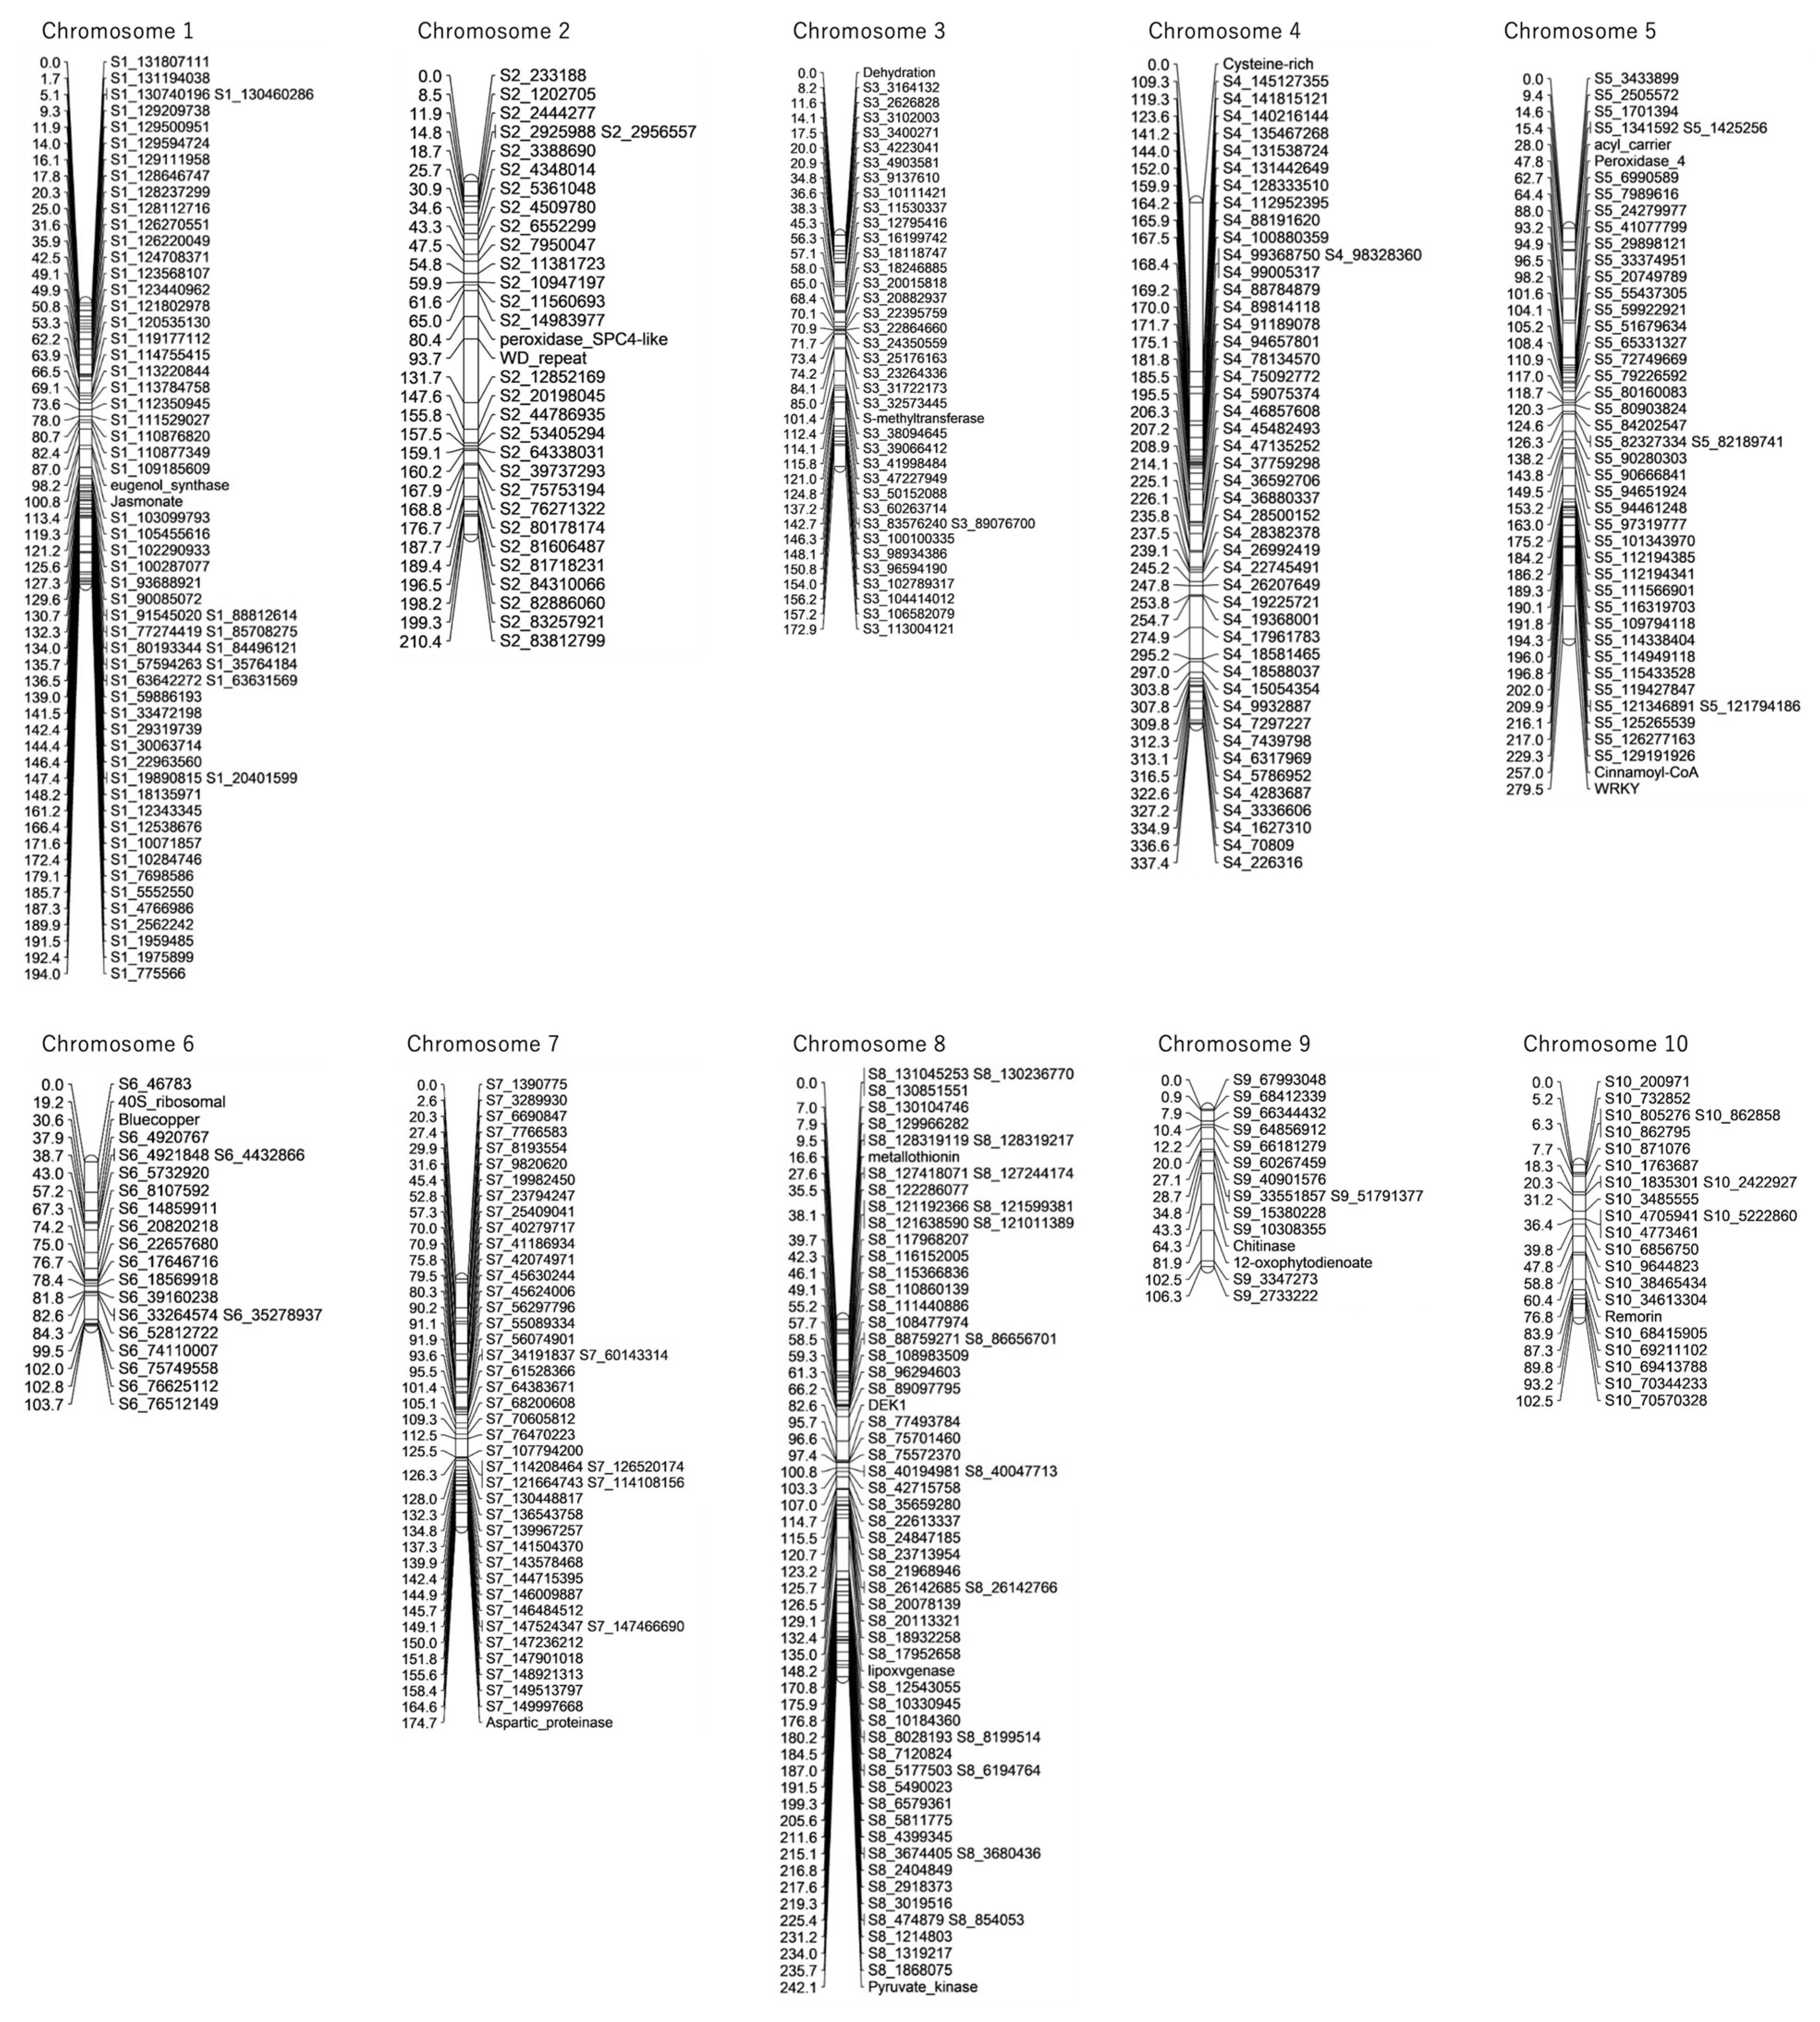
The integrated analysis with 122 individuals (Figure 4) yielded a detailed and high-density map with 402 loci, including 21 RNA-seq-derived markers, across 10 linkage groups spanning 1923 cM, with an average density of 4.78 cM per marker. The grouping of SNP and RNA-seq-derived markers was consistent with that obtained from the WC-9f × OK014 population alone (Figure S1), demonstrating that population integration enhances both the resolution and accuracy of linkage mapping.

3.2.3. QTL Analysis

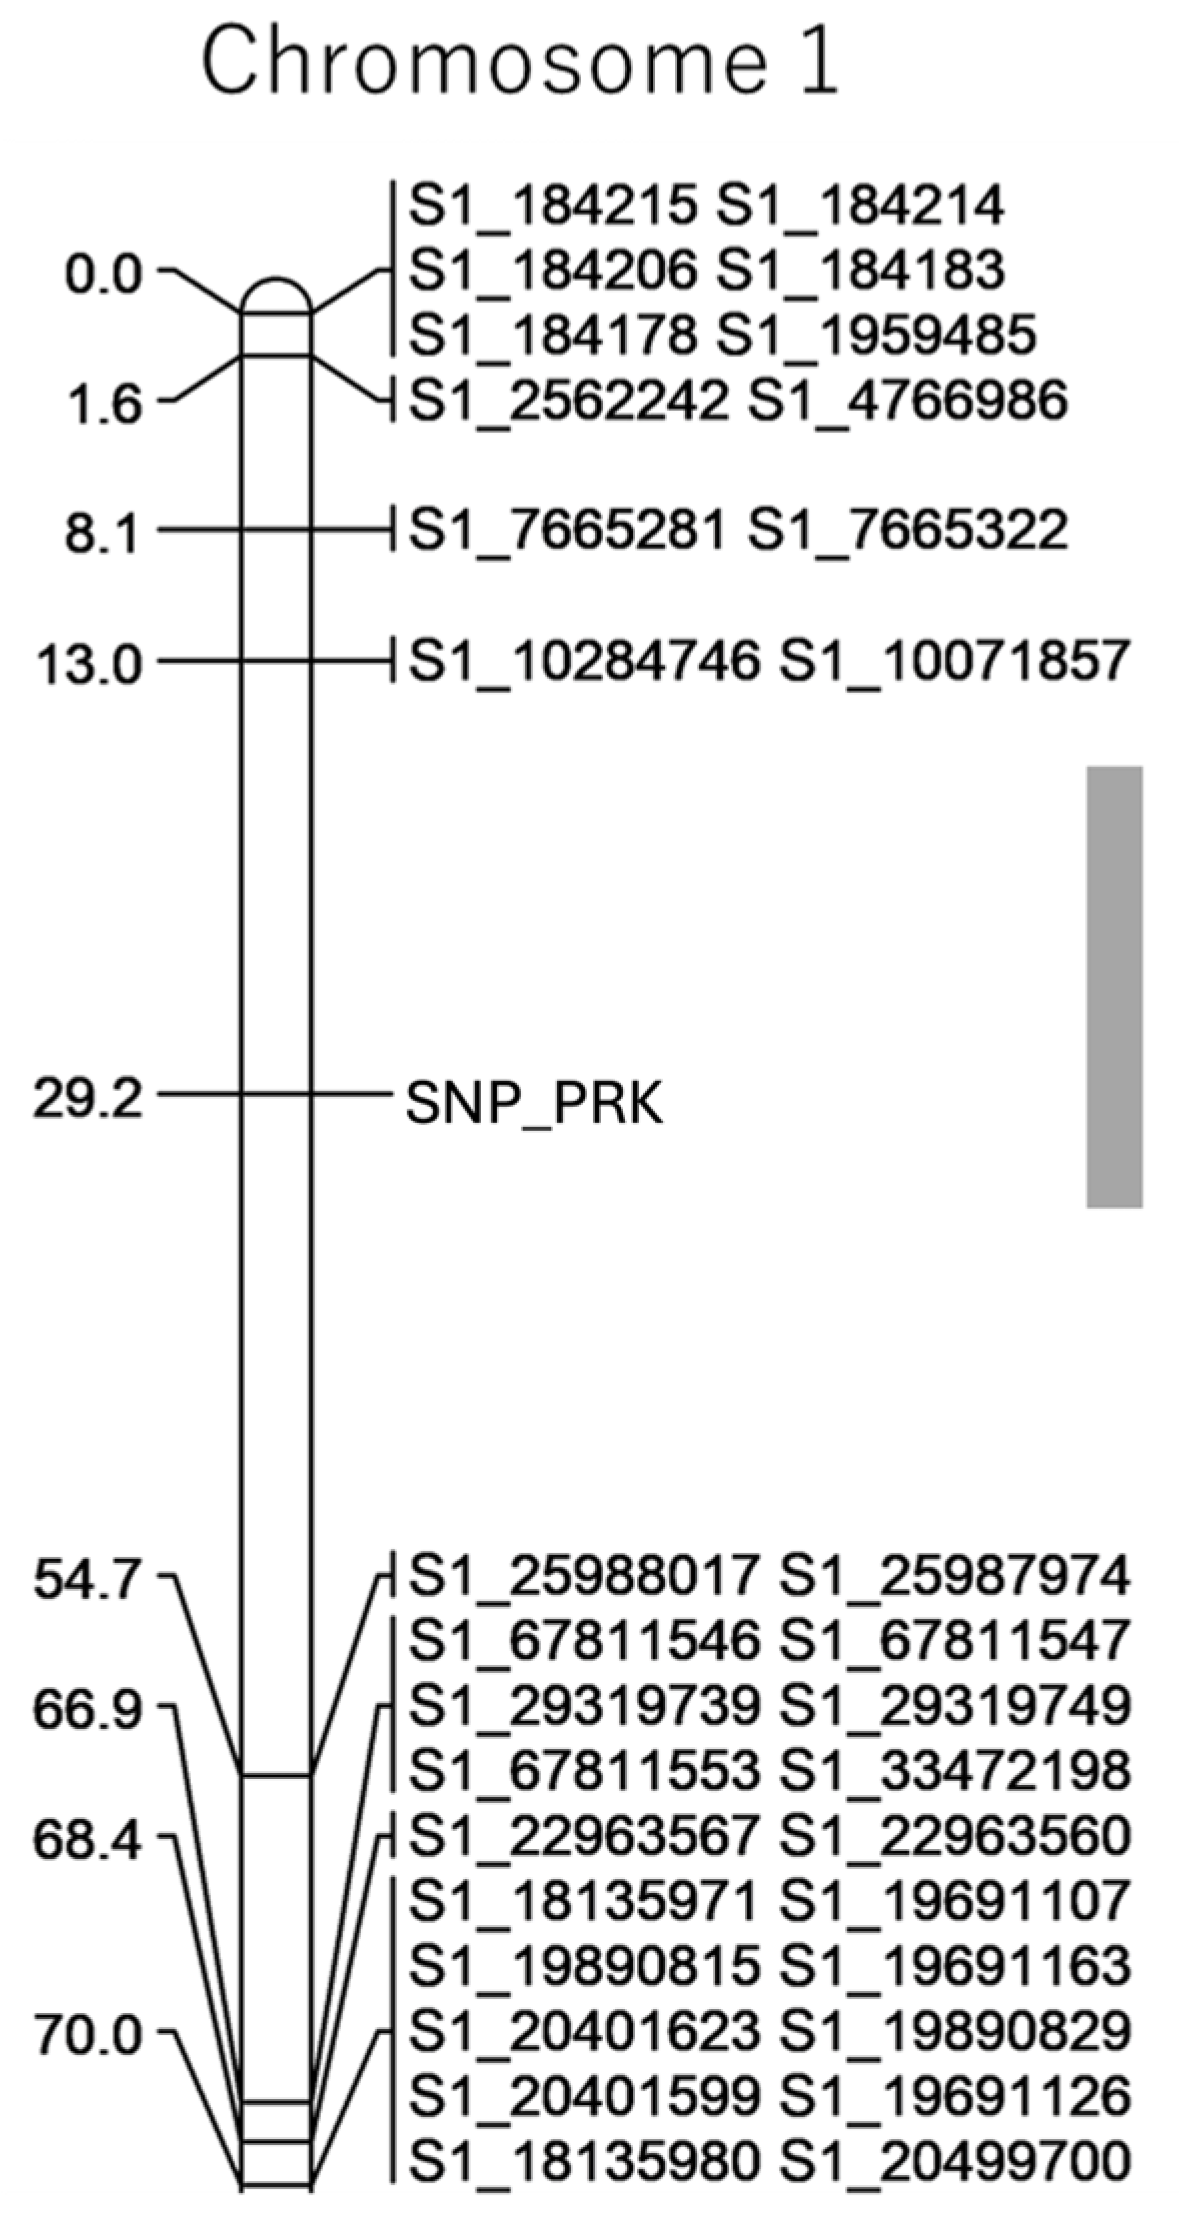
QTL analysis was performed using MapQTL based on the linkage map constructed for the WC-9f × OK014 population (Figure S1). A major QTL associated with resistance to asparagus stem blight was detected on chromosome 1, with a maximum LOD score of 3.68. This QTL explained 13.5% of the phenotypic variation and was located within a confidence interval of 17.2–58.6 cM, with an estimated additive effect of 0.446. SNP_PRK showed a significant association with stem blight resistance within this QTL region (Figure 5).

3.2.4. Development of dCAPS (PRK) and CAPS (PR1) Markers for Stem Blight Resistance

To enable practical marker-assisted selection, a dCAPS marker was developed based on SNP_PRK. Asparagus produced a band at 119 bp, A. kiusianus produced a band at 153 bp, and the interspecific hybrid OK014 exhibited both, corresponding to the 119 bp band from asparagus and the 153 bp band from A. kiusianus. The heterozygous (119/153) was defined as individuals predicted to carry a heterozygous allele, consisting of the asparagus-derived (119 bp) and A. kiusianus-derived (153 bp) alleles. The asparagus type was defined as individuals predicted to possess the asparagus-derived allele in the homozygous state.
Screening of 66 individuals in the BC1 population revealed that, without the marker, resistant and susceptible individuals appeared in nearly equal proportions (34:32), consistent with the expected 1:1 segregation ratio (χ2 = 0.061, df = 1, p = 0.806). When heterozygous individuals carrying the A. kiusianus-derived allele were selected, 23 of 29 (~80%) exhibited resistance (Table 2). Among the 34 resistant individuals, 23 carried the resistance-associated heterozygous genotype, corresponding to a sensitivity of 67.6% (23/34). Among the 32 susceptible individuals, 26 had the asparagus-type genotype, corresponding to a specificity of 81.3% (26/32). Furthermore, the PRK marker genotype also segregated in a 1:1 ratio (29:37; χ2 = 0.970, df = 1, p = 0.325), with a Chi-square independence test confirming that this association was statistically significant (χ2 = 16.0, df = 1, p < 0.0001; Cramér’s V = 0.492). Among the four possible contiguous binary divisions of the five-level DSG scale, the DSG 0–2/3–4 cutoff showed the largest Cramér’s V, indicating the strongest observed association with PRK genotype. Exploratory one-dimensional k-means clustering (k = 2), performed using only the DSG scores and independently of PRK genotype, identified DSG 0–2 and 3–4 as the two-cluster partition with the minimum total WCSS (20.233). These results support the cutoff between DSG 2 and 3, and furthermore, the PRK marker shows potential utility for selecting resistant individuals in breeding programs.
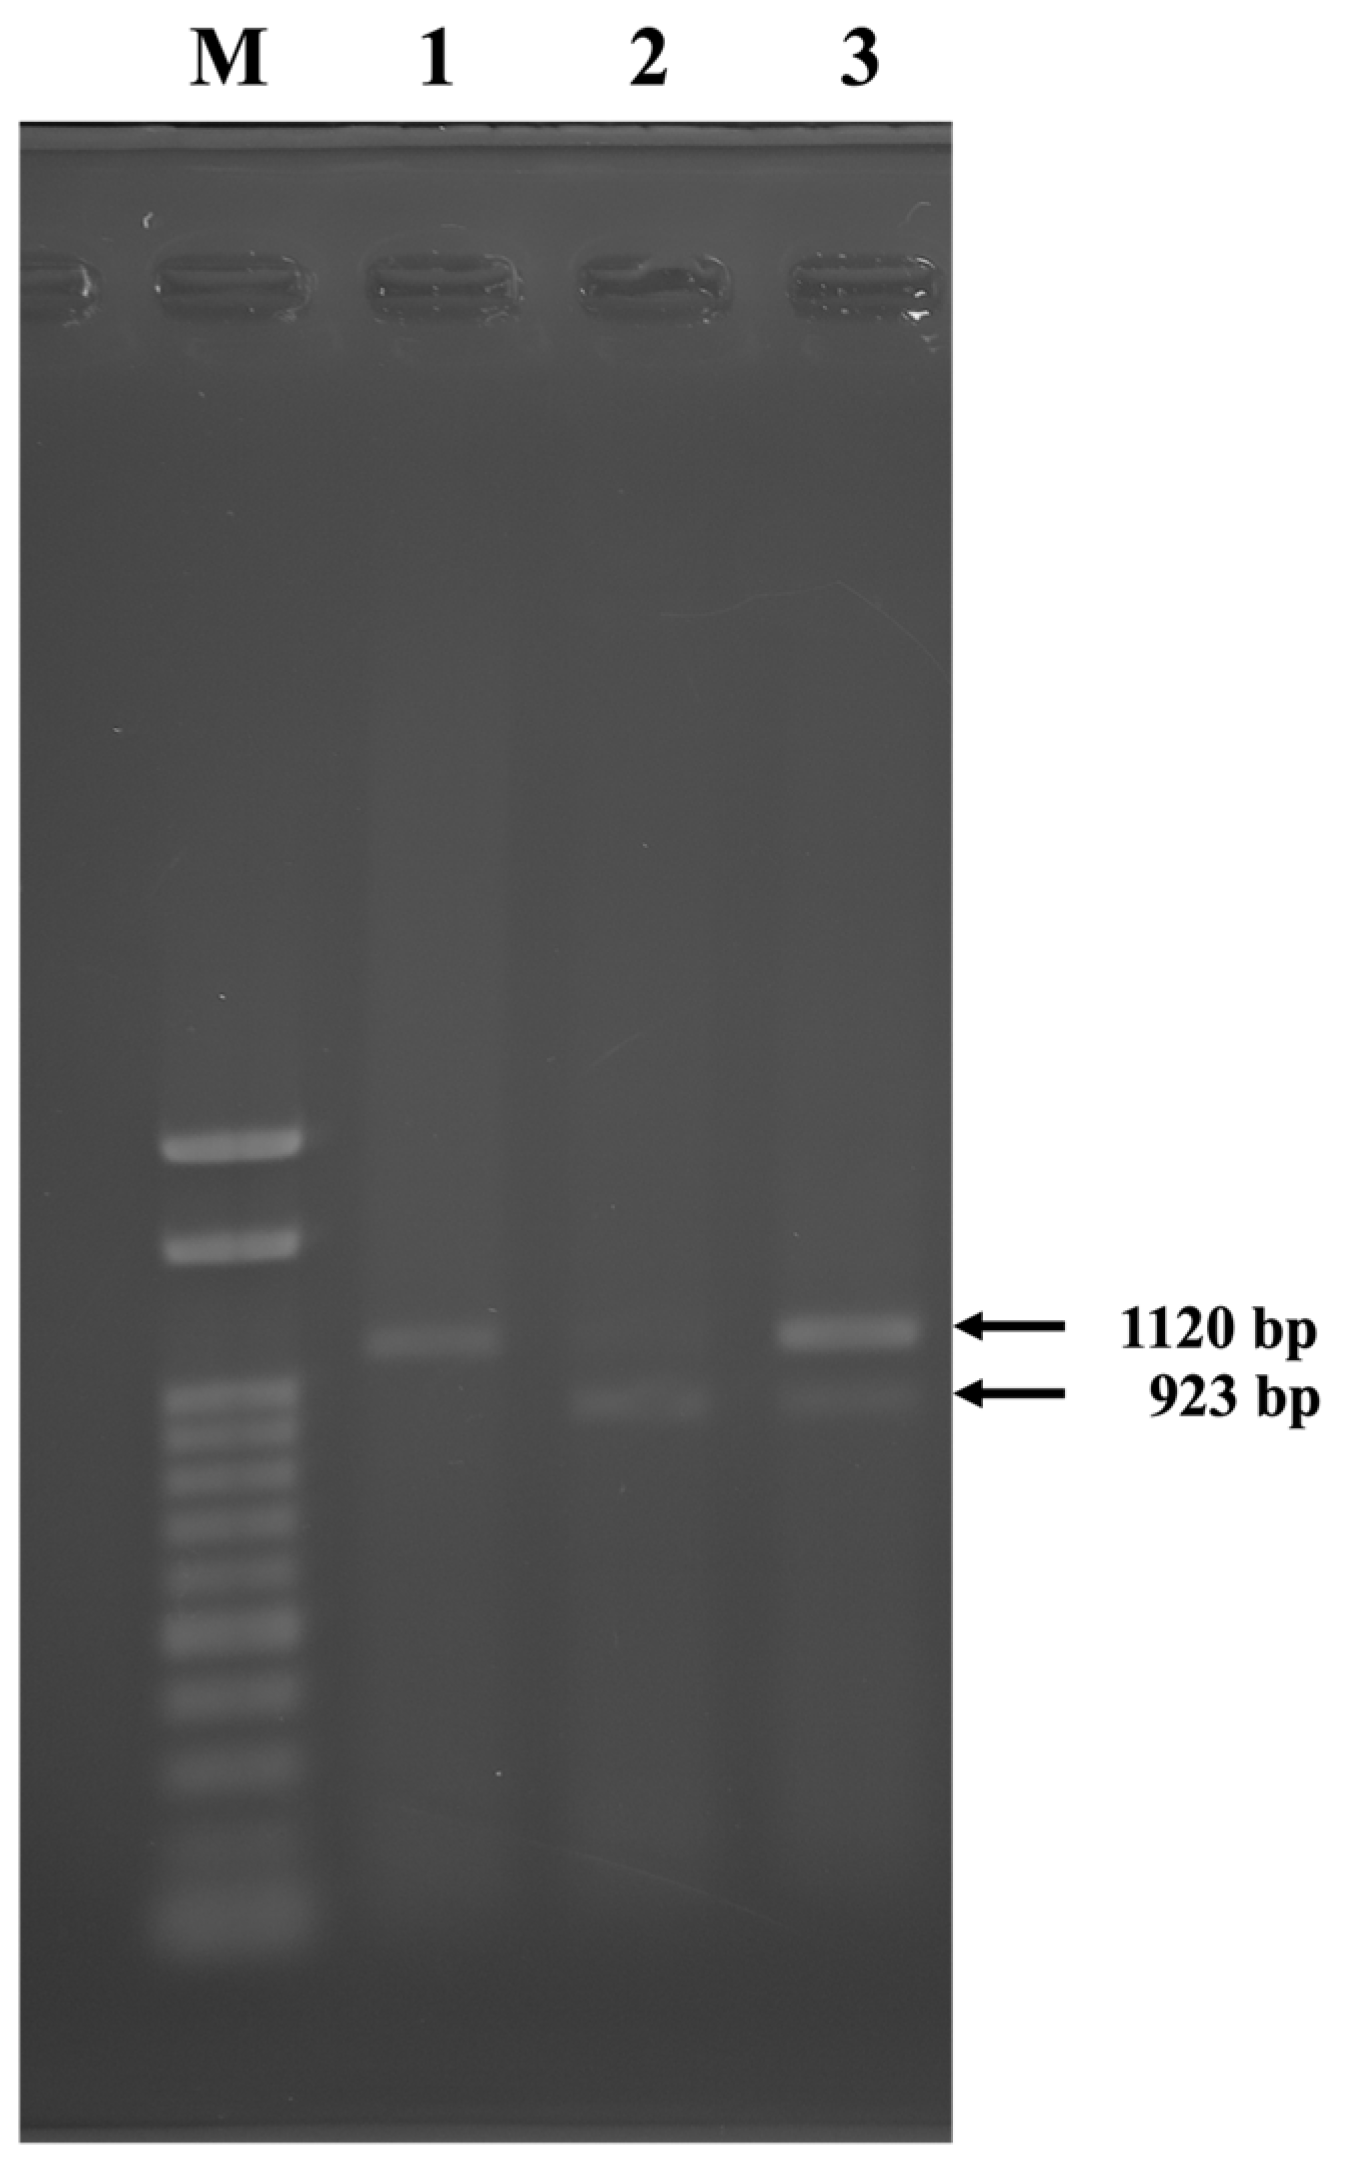
Following PCR amplification with the PR1 marker, the amplicons were digested with XbaI and analyzed using agarose gel electrophoresis (Figure 6). In A. officinalis, a single 1120 bp band was detected, corresponding to the asparagus-derived susceptibility marker. In contrast, A. kiusianus showed a 923 bp band digested from the 1120 bp amplicons, corresponding to the A. kiusianus-derived resistance marker. The interspecific hybrid OK014 exhibited both bands, namely the A. officinalis-derived susceptibility marker (1120 bp) and the A. kiusianus-derived resistance marker (923 bp). The results of the PR1 marker for asparagus and heterozygous types were the same as those obtained with the PRK marker.

4. Discussion

The results of the mating experiment to produce BC1 individuals showed that the fruit set rates ranged from 49.0 to 68.9% for asparagus × F1, which are higher than the values reported for the direct interspecific cross A. officinalis (seed parent) × A. kiusianus (pollen parent), for which fruit sets were only 17.8% [22] and 9.0% [6]. Generally, even if the F1 hybrids show normal growth, poor growth, sterility, or issues such as death and weakness may occur in the F2 generation onward. However, according to the results of this experiment, no such problems were observed in the back-crossed progeny from interspecific hybridization between asparagus and A. kiusianus; therefore, it is unlikely that hybrid fertility issues will arise in future back-cross hybridizations.
In the control asparagus plants inoculated on 18 March and 1 June 2016, the aboveground stems of all individuals took 7 and 11 weeks, respectively, to completely die. Previous studies using a similar inoculation procedure reported that the aboveground stems of most asparagus plants died within approximately 5 weeks after inoculation [7]. However, even in this experiment, a few individuals exhibited incomplete wilting of the stems five weeks after inoculation. Comparing the current results to these earlier reports, it took a notably longer time for the aboveground stems of asparagus to die, and it was thought that pathogen infectivity had decreased due to successive subculture. Defined as the transfer of a small inoculum from an existing culture into fresh sterile medium, subculturing is widely employed for short-term microbial preservation [23]. Some pathogenic fungi show attenuated virulence in response to environmental shifts or extended serial passaging on rich laboratory media [24]. The inoculum used in this study as well as the previous one was the P1 strain of Phomopsis asparagi, preserved at Kyushu University. This strain, collected from Saga Prefecture, was maintained by subculturing. The pathogen’s pathogenicity and infectivity may have decreased during successive subculturing, which is thought to have caused the delayed disease onset in the control asparagus plants compared to previous reports. Such a reduction in virulence may influence phenotypic evaluation by delaying symptom development and introducing variability in disease progression among individuals. A similar phenomenon was reported in Botrytis cinerea, where virulence declined with time in culture and was restored after inoculation on Arabidopsis thaliana [25]. In the resistance test conducted on 18 November 2016, the pathogen from the successively subcultured strain was first inoculated into asparagus, reisolated, and then used as the inoculum. As previously reported, infected stems of asparagus died within 5 weeks, indicating that the infectivity of the inoculum used in the tests on 18 March and 1 June 2016, had declined. These results indicate that Phomopsis asparagi virulence may decline during successive subculturing, leading to delayed disease development in inoculated plants. In the present study, virulence was effectively restored by inoculation onto asparagus stems followed by reisolation, as evidenced by the shortened time to stem death in the November 2016 experiment. Therefore, for accurate phenotypic evaluation of disease resistance, it is recommended to use virulence-restored strains obtained through host passage, or to carefully standardize disease assessment based on symptom progression in control plants, which would minimize the potential bias caused by variation in pathogen infectivity. However, systematic data on virulence stability across subculture generations were not collected in this study; instead, the use of control plants as an internal reference provided a practical means of accounting for such variation across experimental batches. In this context, evaluating disease symptoms based on symptom progression in the control asparagus plants, rather than relying solely on fixed days post-inoculation, is more appropriate, particularly when pathogen virulence may vary. Comparing disease symptoms among individuals in the BC1 population at the point when half of the control asparagus plants had died and when all had died revealed similar segregation patterns of resistance and susceptibility, suggesting that resistance evaluation can be conducted at an earlier stage when approximately 50% of the control plants have died, while retaining a broadly similar population-level DSG distribution. For future studies, the use of low-passage or freshly isolated pathogen strains, periodic host passage to restore virulence, and standardization of inoculum quality are recommended to ensure more consistent phenotypic evaluation.
Three individuals in the WC-9f × OK014 cross showed a disease severity grade of 0 at the end of the resistance test (Figure 3b). It is difficult to determine whether these individuals possess strong disease resistance or if the observed reduction in fungal strain infectivity is involved at this stage. Furthermore, differences in plant growth conditions at the time of inoculation may also have influenced disease occurrence; these factors should be verified in future studies.
The inoculation assay itself also has some limitations, as it is partially destructive, and severely susceptible plants may exhibit complete dieback of aerial stems or even plant death after inoculation. Although biological replicates could be obtained through plant division prior to inoculation, such treatment may result in differences in plant growth conditions and physiological status, variability which would reduce the uniformity of experimental conditions. Although the disease progression rate differed among the inoculation experiments, susceptible control plants included in each experiment provided an internal reference for determining a comparable biological stage for disease assessment. Furthermore, previous studies repeatedly evaluated A. officinalis UC157F1, A. kiusianus, and their F1 hybrids by inoculation assays in 2011 and 2012, and consistent resistance results were obtained [7], suggesting that this assay can provide consistent resistance results across repeated evaluations.
In general, major gene control is expected to produce a bimodal distribution, whereas polygenic control is expected to produce a unimodal distribution. The resistance segregation patterns observed in the BC1 populations in this study could be classified into two distinct types. As shown in Figure 7, in the WC-9f × OK014 cross, the numbers of plants with disease severity grades 2 and 4 were higher than those in the other grades, indicating the separation of resistant and susceptible individuals into two distinct groups, DSG 0–2 and 3–4, suggesting that the stem blight disease resistance in OK014 is likely controlled by major genes. In contrast, in the crosses WC-9f × OK007, WC2 × WCK3, and OK011 × KAG WC No. 28, a unimodal distribution was observed, with disease severity grade 4 as the peak, indicating that the stem blight disease resistance in their parental F1 hybrids may be under polygenic control. Previous studies on rice blast disease have reported genes that provide strong resistance to rice blast on their own, as well as those that show an accumulation effect when combined with other resistance genes [26]. The results of this experiment suggest that both major genes and polygenic control are involved in the resistance to asparagus stem blight identified in A. kiusianus. In all three crosses exhibiting polygenic control, the majority of individuals showed disease severity grade 4, indicating susceptibility. Since the resistance inoculation test in this study was conducted under conditions that favored pathogen infection, such as high humidity, and these conditions were harsher than the plants’ actual growth environment, the resistance distribution may have been skewed toward susceptibility.
In the WC-9f × OK014 and WC-9f × OK007 crosses, the contrasting resistance segregation patterns suggest possible genetic differences between the two F1 male parents. Based on the RAD-seq genotype data used for linkage map construction, both OK014 and OK007 were classified as heterozygous np at the SNP_PRK locus. Although OK014 and OK007 originated from the same parental cross (AO0060F × AK0501M), the actual resistance gene has not yet been identified and may be linked to the SNP_PRK locus; therefore, although the two F1 individuals had the same SNP_PRK genotype, they may have inherited different alleles at the actual resistance locus. One possibility is that AK0501 was heterozygous at the actual resistance locus, resulting in resistance-associated allele transmission to one F1 individual but not to the other. Alternatively, recombination between SNP_PRK and the actual resistance locus during gamete formation in AK0501 may have separated the marker allele from the linked resistance-associated allele in one of the F1 individuals. QTL analysis based on the OK014-derived linkage map identified a major resistance locus on chromosome 1 (LOD = 3.68). Among BC1 individuals carrying the A. kiusianus-derived allele at this locus, approximately 80% exhibited resistance, indicating its strong effect and being consistent with the bimodal distribution observed in the WC-9f × OK014 population. In contrast, the WC-9f × OK007 population showed a unimodal distribution skewed toward higher disease severity grades, which did not allow for clear classification into resistant and susceptible groups. This phenotypic pattern suggests that resistance in the WC-9f × OK007 population may be under polygenic control and governed by multiple loci with smaller additive effects. Although OK007 was classified as heterozygous np at SNP_PRK, the genotype at the putative causal resistance locus underlying the chromosome 1 QTL and the surrounding haplotypes were not determined; therefore, we cannot determine whether OK007 and OK014 carry the same resistance-associated allele at this locus. Furthermore, the possible involvement of susceptibility-promoting genes analogous to those identified in rice [27], which may be differentially distributed between OK014 and OK007, cannot be excluded and warrants investigation in future studies employing diverse cross combinations. These results suggest that while OK014 and OK007 share a broadly similar genomic background, major gene inheritance and polygenic control may differ between their respective BC1 populations, a difference which may be associated with the contrasting resistance segregation patterns observed between the two crosses.
In this study, we successfully developed SNP markers associated with stem blight disease resistance in asparagus by integrating RAD sequencing, linkage map construction, and QTL analysis. Previous genetic studies in asparagus have been largely confined to sex determination, with no molecular investigation addressing disease resistance [16]. Furthermore, although SNP markers in asparagus have been reported, the resulting linkage maps remain sparse [15], limiting their utility for QTL-based trait dissection. In the present study, we address these gaps by integrating RADseq-based high-density linkage map construction with QTL analysis, leading to the identification of a major resistance locus on chromosome 1 and the development of a codominant CAPS marker (PR1) with potential value for marker-assisted selection in asparagus breeding programs.
The identification of over 3000 SNPs in the WC-9f × OK014 and WC-9f × OK007 populations, including a significant proportion derived from A. kiusianus, highlights RADseq’s effectiveness in capturing polymorphisms from interspecific backgrounds.
The integration of the two BC1 populations (WC-9f × OK014 and WC-9f × OK007) increased the amount of information available for linkage map construction. OK014 and OK007 are full-sib F1 individuals derived from the same A. officinalis × A. kiusianus cross and therefore share part, although not all, of their genetic composition. Accordingly, only loci showing the same nn × np genotype pattern in both crosses and for which the p allele was derived from A. kiusianus were used to construct the integrated linkage map. This integration enabled all RNA-seq-derived markers to be successfully mapped. Joint linkage analysis of related populations sharing a common parent has also been shown to increase mapping power compared with separate analyses of individual families [28]; however, in the present study, the two populations were combined only for linkage map construction and not for joint QTL analysis.
Formal population-structure analyses and statistical comparisons of allele frequencies between the two BC1 populations were not conducted before integration; therefore, family-specific differences in allele frequencies, segregation ratios, or recombination frequencies cannot be completely excluded and should be examined in future studies.
A major QTL for stem blight disease resistance was consistently identified on chromosome 1, with SNP_PRK demonstrating a strong association (LOD > 3). SNP markers are widely used in genetic diversity assessments, molecular evolution studies, and agronomically important trait mapping in crop species. While SNP assays often require expensive equipment or reagents, the conversion to more accessible marker systems, such as dCAPS, offers a simpler and more cost-effective alternative. Derived cleaved amplified polymorphic sequence (dCAPS) markers detect SNPs by introducing mismatches into one PCR primer flanking the polymorphism, which creates or abolishes a restriction enzyme recognition site in one haplotype, a method widely used in plant molecular genetics [29,30,31]. Screening of 66 individuals in the BC1 population revealed that when heterozygous individuals carrying the A. kiusianus-derived allele were selected, 23 of 29 individuals (~80%) exhibited resistance. These results suggest that SNP_PRK has potential value for selecting resistant individuals within the population examined. However, in some asparagus samples, the banding pattern generated by the dCAPS assay was occasionally unstable; therefore, a CAPS marker was further developed to achieve more stable and consistent genotyping.
The CAPS marker system, also referred to as PCR–RFLP, combines PCR amplification with restriction enzyme digestion, offering a more rapid and less labor-intensive alternative to conventional Southern blot-based RFLP analysis [32]. One of the most important advantages of CAPS markers is their codominant nature, which allows clear discrimination between homozygous and heterozygous individuals, making them particularly useful for detailed genetic analyses [33].
In the present study, XbaI digestion of the CAPS marker PR1 produced a clear polymorphic pattern: a 1120 bp band in A. officinalis, a 923 bp fragment in A. kiusianus, and both bands in the interspecific hybrid OK014. The results were consistent with those obtained using the PRK marker, suggesting that PR1 is a potentially useful marker for stem blight resistance selection in asparagus breeding.
Although gene expression analysis was not performed in the present study, we compared the position of the PR1 marker with 21 resistance-related genes previously reported by Abdelrahman et al. [6]. Among these, two were located on the same chromosome as the PR1 marker but were genetically distant from it and therefore were not considered to be closely linked to the PR1 marker. Thus, the present genetic map information does not support a direct relationship between the PR1 marker and these previously reported resistance-related genes. Further fine mapping, expression analysis, and functional validation will be required in future studies to identify the causal gene or genes underlying the observed resistance.
These findings suggest that PR1 may serve as a complementary tool alongside time-consuming field inoculation tests, with potential to improve stem blight resistance breeding efficiency in asparagus. Further validation using larger and more diverse populations will be required to determine its robustness and general applicability.

5. Conclusions

In this study, we investigated the inheritance of stem blight resistance in BC1 populations derived from interspecific crosses between Asparagus officinalis and A. kiusianus and developed a molecular marker applicable to marker-assisted selection. The resistance segregation patterns observed in the BC1 populations varied depending on the cross combination, suggesting that both major gene and polygenic control are involved in stem blight resistance in A. kiusianus. In particular, the bimodal segregation pattern observed in the WC-9f × OK014 population indicated the involvement of a major resistance gene in OK014.
Using RAD sequencing, a total of 3393 SNPs were identified, and an integrated linkage map of 402 loci was constructed by combining two BC1 populations, which improved marker density and map resolution compared with single-population mapping. QTL analysis identified a major resistance locus on chromosome 1, with SNP_PRK showing a significant association (LOD > 3). Genotyping with a dCAPS marker developed from this SNP showed that approximately 80% of heterozygous individuals exhibited resistance. The CAPS marker PR1 distinguished the A. officinalis- and A. kiusianus-derived and heterozygous genotypes, producing results consistent with those obtained using PRK in the evaluated materials.
PR1 may therefore be useful for selecting resistant individuals in breeding programs, acting as a complementary tool to phenotypic evaluation. Further validation in independent and genetically diverse populations will be required to assess its broader applicability.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/horticulturae12080953/s1, Figure S1: Genetic map using WC-9f × OK014 (68 individuals). (No. of loci: 337, No. of linkage groups: 10, Map distance: 1813 cM, Average marker density: 5.38 cM/marker).

Author Contributions

Conceptualization, T.I., A.U., S.-i.W. and Y.O.; methodology, Y.T., E.K. (Emika Kakizoe), E.K. (Eri Kato) and M.M. (Masaru Matsumoto); software, Y.T. and Y.Y.; validation, J.-i.M., Y.M., K.S., M.A., A.K., T.I., M.M. (Mitsutaka Mori) and K.M.; formal analysis, Y.L., Y.T. and Y.Y.; resources, K.T.; draft preparation, Y.L. and Y.O.; writing—review and editing, M.M. (Masaru Matsumoto), Y.Y., A.K., T.I. and Y.O.; visualization, Y.L., Y.T. and E.K. (Emika Kakizoe); supervision, Y.O.; project administration, A.U. and S.-i.W. All authors have read and agreed to the published version of the manuscript.

Funding

This work was supported by a Grant-in-Aid for Science and Technology Research Promotion Program (27002B) for Agriculture, Forestry, Fisheries and Food Industry from the Ministry of Agriculture, Forestry and Fisheries (MAFF) (Japan), by the Research Program on Development of Innovative Technology Grants (JPJ007097) from the Project of the Bio-oriented Technology Research Advancement Institution (BRAIN), and by the Research and Implementation Promotion Program through Open Innovation Grants (JPJ011937) from the Project of the BRAIN.

Data Availability Statement

The original contributions presented in this study are included in the article/Supplementary Materials. Further inquiries can be directed to the corresponding authors.

Acknowledgments

We gratefully thank M. Shigyo at Yamaguchi University and Y. Monden at Okayama University for providing useful information regarding RAD sequencing and integrated analyses in dioecious plants.

Conflicts of Interest

The authors declare no conflict of interest.

References

  1. Guo, Q.; Wang, N.; Liu, H.; Li, Z.; Lu, L.; Wang, C. The bioactive compounds and biological functions of Asparagus officinalis L.—A review. J. Funct. Foods 2020, 65, 103727. [Google Scholar] [CrossRef] [Scilit]
  2. Sakai, Y. Disorders and Countermeasures in Asparagus. In Agricultural Technology System, Vegetable Section 8-②: Asparagus, Basic Edition; Rural Culture Association Japan: Tokyo, Japan, 1986; pp. 237–239. (In Japanese) [Google Scholar]
  3. Kobayashi, M.; Shinsu, T. Rain shelter cultivation of green asparagus. Bull. Nagasaki Pref. Agric. For. Exp. Stn. Agric. Div. 1990, 18, 117–145, (In Japanese with English Summary). [Google Scholar]
  4. Sonoda, T.; Uragami, A.; Ito, K.; Kohmura, H.; Ohwada, M.; Kaji, K. Evaluation of Asparagus species and comparison between sexes in A. officinalis cultivars for resistance to stem blight. J. Jpn. Soc. Hortic. Sci. 2001, 70, 244–250, (In Japanese with English Summary). [Google Scholar]
  5. Kanno, A.; Yokoyama, J. Asparagus. In Wild Crop Relatives: Genomic and Breeding Resources; Kole, C., Ed.; Springer: Berlin/Heidelberg, Germany, 2011; pp. 23–42. [Google Scholar] [CrossRef] [Scilit]
  6. Abdelrahman, M.; Suzumura, N.; Mitoma, M.; Matsuo, S.; Ikeuchi, T.; Mori, M.; Murakami, K.; Ozaki, Y.; Matsumoto, M.; Uragami, A.; et al. Comparative de novo transcriptome profiles in Asparagus officinalis and A. kiusianus during the early stage of Phomopsis asparagi infection. Sci. Rep. 2017, 7, 2608. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Iwato, M.; Kosaza, M.; Takeuchi, Y.; Matsumoto, M.; Inada, M.; Ozaki, Y.; Okubo, H. Stem blight resistance of Asparagus kiusianus and its hybrid with A. officinalis. Adv. Hortic. Sci. 2014, 28, 202–207. [Google Scholar] [CrossRef] [Scilit]
  8. Takeuchi, Y.; Kakizoe, E.; Yoritomi, R.; Iwato, M.; Kanno, A.; Ikeuchi, T.; Mori, M.; Murakami, K.; Uragami, A.; Matsumoto, M.; et al. Features in stem blight resistance confirmed in interspecific hybrids of Asparagus officinalis L. and Asparagus kiusianus Makino. Hortic. J. 2018, 87, 200–205. [Google Scholar] [CrossRef] [Scilit]
  9. Elshire, R.J.; Glaubitz, J.C.; Sun, Q.; Poland, J.A.; Kawamoto, K.; Buckler, E.S.; Mitchell, S.E. A robust, simple genotyping-by-sequencing (GBS) approach for high diversity species. PLoS ONE 2011, 6, e19379. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Baird, N.A.; Etter, P.D.; Atwood, T.S.; Currey, M.C.; Shiver, A.L.; Lewis, Z.A.; Selker, E.U.; Cresko, W.A.; Johnson, E.A. Rapid SNP discovery and genetic mapping using sequenced RAD markers. PLoS ONE 2008, 3, e3376. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Barchi, L.; Lanteri, S.; Portis, E.; Acquadro, A.; Valè, G.; Toppino, L.; Rotino, G.L. Identification of SNP and SSR markers in eggplant using RAD tag sequencing. BMC Genom. 2011, 12, 304. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Melaku, G.; Guangfu, H.; Shilai, Z.; Labroo, M.; Rhodes, B.; Harold, E.; Hu, F. Single marker analysis for leaf gas exchange traits from RILS of RD 23 (O. sativa L.) and O. longistaminata. Biotechnol. Rep. 2022, 35, e00743. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Wang, L.; Conteh, B.; Fang, L.; Xia, Q.; Nian, H. QTL mapping for soybean (Glycine max L.) leaf chlorophyll-content traits in a genotyped RIL population by using RAD-Seq based high-density linkage map. BMC Genom. 2020, 21, 739. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Volynkin, V.; Vasylyk, I.; Volodin, V.; Grigoreva, E.; Karzhaev, D.; Lushchay, E.; Ulianich, P.; Volkov, V.; Risovannaya, V.; Blinova, S.; et al. The assessment of agrobiological and disease resistance traits of grapevine hybrid populations (Vitis vinifera L. × Muscadinia rotundifolia Michx.) in the climatic conditions of Crimea. Plants 2021, 10, 1215. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Mercati, F.; Riccardi, P.; Leebens-Mack, J.; Abenavoli, M.R.; Falavigna, A.; Sunseri, F. Single nucleotide polymorphism isolated from a novel EST dataset in garden asparagus (Asparagus officinalis L.). Plant Sci. 2013, 203–204, 115–123. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. Moreno, R.; Castro, P.; Vrána, J.; Kubaláková, M.; Cápal, P.; García, V.; Gil, J.; Millán, T.; Doležel, J. Integration of genetic and cytogenetic maps and identification of sex chromosome in garden asparagus (Asparagus officinalis L.). Front. Plant Sci. 2018, 9, 1068. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Bock, C.H.; Poole, G.H.; Parker, P.E.; Gottwald, T.R. Plant disease severity estimated visually, by digital photography and image. analysis, and by hyperspectral imaging. Crit. Rev. Plant Sci. 2010, 29, 59–107. [Google Scholar] [CrossRef] [Scilit]
  18. Shaner, G.; Finney, R.E. The effect of nitrogen fertilization on the expression of slow-mildewing resistance in Knox wheat. Phytopathology® 1977, 67, 1051–1056. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Dellaporta, S.L.; Wood, J.; Hicks, J.B. A Plant DNA Minipreparation: Version II. Plant Mol. Biol. Rep. 1983, 1, 19–21. [Google Scholar] [CrossRef] [Scilit]
  20. Poland, J.A.; Brown, P.J.; Sorrells, M.E.; Jannink, J.-L. Development of high-density genetic maps for barley and wheat using a novel two-enzyme genotyping-by-sequencing approach. PLoS ONE 2012, 7, e32253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Abdelrahman, M.; Nakabayashi, R.; Mori, T.; Ikeuchi, T.; Mori, M.; Murakami, K.; Ozaki, Y.; Matsumoto, M.; Uragami, A.; Tsujimoto, H.; et al. Comparative metabolome and transcriptome analyses of susceptible Asparagus officinalis and resistant wild A. kiusianus reveal insights into stem blight disease resistance. Plant Cell Physiol. 2020, 61, 1464–1476. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Ito, T.; Konno, I.; Kubota, S.; Ochiai, T.; Sonoda, T.; Hayashi, Y.; Fukuda, T.; Yokoyama, J.; Nakayama, H.; Kameya, T.; et al. Production and characterization of interspecific hybrids between Asparagus kiusianus Makino and A. officinalis L. Euphytica 2011, 182, 285–294. [Google Scholar] [CrossRef] [Scilit]
  23. Senaratne, W.M.T.N.; Jayaweera, J.A.A.S. Comparison of microbial preservation methods: A narrative review. Germs 2024, 14, 375–386. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Tini, F.; Beccari, G.; Marconi, G.; Porceddu, A.; Sulyok, M.; Gardiner, D.M.; Albertini, E.; Covarelli, L. Identification of putative virulence genes by DNA methylation studies in the cereal pathogen Fusarium graminearum. Cells 2021, 10, 1192. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  25. Breen, J.; Mur, L.A.J.; Sivakumaran, A.; Akinyemi, A.; Wilkinson, M.J.; Rodriguez Lopez, C.M. Botrytis cinerea loss and restoration of virulence during in vitro culture follows flux in global DNA methylation. Int. J. Mol. Sci. 2022, 23, 3034. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Yasuda, N.; Mitsunaga, T.; Hayashi, K.; Koizumi, S.; Fujita, Y. Effects of pyramiding quantitative resistance genes Pi21, Pi34, and Pi35 on rice leaf blast disease. Plant Dis. 2015, 99, 904–909. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Fukuoka, S.; Yamamoto, S.-I.; Mizobuchi, R.; Yamanouchi, U.; Ono, K.; Kitazawa, N.; Yasuda, N.; Fujita, Y.; Nguyen, T.T.T.; Koizumi, S.; et al. Multiple functional polymorphisms in a single disease resistance gene in rice enhance durable resistance to blast. Sci. Rep. 2014, 4, 4550. [Google Scholar] [CrossRef] [Scilit]
  28. Li, H.; Bradbury, P.; Ersoz, E.; Buckler, E.S.; Wang, J. Joint QTL linkage mapping for multiple-cross mating design sharing one common parent. PLoS ONE 2011, 6, e17573. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Neff, M.M.; Turk, E.; Kalishman, M. Web-based primer design for single nucleotide polymorphism analysis. Trends Genet. 2002, 18, 613–615. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Neff, M.M.; Neff, J.D.; Chory, J.; Pepper, A.E. dCAPS, a simple technique for the genetic analysis of single nucleotide polymorphisms: Experimental applications in Arabidopsis thaliana genetics. Plant J. 1998, 14, 387–392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Michaels, S.D.; Amasino, R.M. A robust method for detecting single-nucleotide changes as polymorphic markers by PCR. Plant J. 1998, 14, 381–385. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. An, H.; Lee, H.-Y.; Shim, D.; Choi, S.H.; Cho, H.; Hyun, T.K.; Jo, I.-H.; Chung, J.-W. Development of CAPS markers for evaluation of genetic diversity and population structure in the germplasm of button mushroom (Agaricus bisporus). J. Fungi 2021, 7, 375. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Kulkarni, K.P.; Appiah, R.K.; Reddy, U.K.; Melmaiee, K. Cleaved amplified polymorphic sequence markers in horticultural crops: Current status and future perspectives. Agronomy 2024, 14, 2598. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Procedure of ligation (A) and PCR (B) for RADseq (modified from [20]).
Horticulturae 12 00953 g001
Figure 2. Number of individuals in each cross combination classified by disease severity grade at different evaluation time points in the inoculation test. (n) Number of individuals tested; (a,a’) WC-9f × OK007; (b,b’) WC-9f × OK014; (c,c’) WC2 × WCK3. (ac) Evaluation performed when a half of the control asparagus plants reached a DSG of 4. (a’c’): Evaluation performed when all control asparagus plants reached a DSG of 4.
Horticulturae 12 00953 g002
Figure 3. Number of BC1 individuals with disease severity grade (DSG) category. (a) WC-9f × OK007; (b) WC-9f × OK014; (c) WC2 × WCK3; (d) OK011 × KAG WC No. 28.
Horticulturae 12 00953 g003
Figure 4. Genetic map using WC-9f × OK014 (68 individuals) and WC-9f × OK007 (54 individuals). (No. of loci: 402, No. of linkage groups: 10, map distance: 1923 cM, average marker density: 4.78 cM/marker).
Horticulturae 12 00953 g004
Figure 5. Linkage map of chromosome 1 showing QTL associated with resistance to asparagus stem blight. Gray bar: LOD > 3 (maximum LOD value: 3.68).
Horticulturae 12 00953 g005
Figure 6. Electrophoretic analysis of the CAPS marker PR1. (M) 100 bp DNA ladder marker; (1) A. officinalis; (2) A. kiusianus; (3) interspecific hybrid OK014.
Horticulturae 12 00953 g006
Figure 7. Resistance segregation patterns in the BC1 populations. (A) WC-9f × OK014. (B) WC-9f × OK007. (C) WC2 × WCK3. (D) OK011 × KAG WC No. 28. The x-axis indicates disease severity grade, and the y-axis indicates the number of BC1 individuals. Disease severity grades 0–2 were classified as resistant, whereas grades 3–4 were classified as susceptible.
Horticulturae 12 00953 g007
Table 1. Results of crosses between asparagus and interspecific hybrid individuals.
Seed ParentPollen ParentNo. of Flowers Used for CrossingNo. of Fruits Set (%) aNo. of Harvested Fruits (%) bNo. of Seeds
Obtained (Mean) c
Germination Rate (%) d
A. officinalis × F1
WC-9fOK0075125 (49.0)21 (41.2)66 (3.1)74.2
WC-9fOK0144531 (68.9)31 (68.9)70 (2.3)84.3
Pooled9656 (58.3)52 (54.2)136 (2.6)79.4
a: Fruit set (%) = (No. of fruits set/No. of flowers used for crossing) × 100; b: Harvested fruits rate (%) = (No. of harvested fruits/No. of flowers used for crossing) × 100; c: No. of seeds per fruit = No. of seeds obtained/No. of harvested fruits; d: Germination rate (%) = (No. of germinated seeds/No. of seeds obtained) × 100.
Table 2. Frequency of resistant and susceptible individuals by dCAPS marker PRK type in the BC1 population.
PRK GenotypeNo. of Individuals (Percentage)Total
DSG: 0DSG: 1DSG: 2DSG: 3DSG: 4
119/153
(Heterozygous type)
35153329 (100) y
23 (79.3) z6 (20.7) z
119/119
(Asparagus type)
011062037 (100) y
11 (29.7) z26 (70.3) z
Total362592366 (100)
34 (51.5) y32 (48.5) y
y: Chi-square goodness-of-fit test for the expected 1:1 segregation ratio: PRK marker genotype, 29:37 (χ2 = 0.970, df = 1, p = 0.325); resistance phenotype (DSG 0–2 vs. DSG 3–4), 34:32 (χ2 = 0.061, df = 1, p = 0.806). z: Chi-square test of independence between PRK marker genotype and resistance phenotype (DSG 0–2 vs. DSG 3–4) (χ2 = 16.0, df = 1, p < 0.0001; Cramér’s V = 0.492). Based on this classification, the sensitivity and specificity of the resistance-associated genotype were 67.6% (23/34) and 81.3% (26/32), respectively.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.