


Abstract
Reproductive barriers severely limit interspecific hybridization success among Hydrangea macrophylla, H. paniculata, and H. arborescens, thereby restricting the combination of ornamental traits and cold hardiness. We evaluated cross-compatibility, pollen tube growth, and embryo development in both direct and reciprocal crosses involving H. macrophylla with H. paniculata and H. arborescens. Both species pairs exhibited pronounced unilateral incompatibilities. When H. macrophylla served as the maternal parent, the percentages of seedling emergence were higher, whereas reciprocal crosses produced >84% ovary swelling but resulted in almost no seedlings. Fluorescence microscopy revealed mild prezygotic barriers in direct crosses but strong inhibition of pollen germination and pollen tube growth in reciprocal crosses. Paraffin section observations showed that postzygotic barriers were the primary cause of hybrid failure, with endosperm-type abortion predominating in direct crosses and embryo-type or complete abortion in reciprocal crosses. Consistent with these abortion patterns, direct crosses maintained higher proportions of normal embryos, whereas reciprocal crosses dropped below 10% at the globular stage and approached 0% at later stages. These findings support the use of timely embryo rescue for direct crosses and targeted mitigation of prezygotic barriers in reciprocal crosses to improve Hydrangea interspecific hybridization efficiency.
1. Introduction
The genus Hydrangea comprises 73 species worldwide. China serves as a primary origin and distribution center, hosting 47 species and 11 varieties, which constitute approximately two-thirds of the global total [1]. Hydrangea species are recognized as one of the three major garden plants globally and are widely used in cut flower production, landscape gardening, and potted plant cultivation [2]. Their appeal stems from their extended flowering duration, large inflorescences, and diverse flower colors [3,4].
Hydrangea possesses abundant germplasm resources and substantial ornamental value; however, contemporary breeding practices face several bottlenecks [5]. Historically, breeding objectives have primarily focused on improving ornamental traits, such as flower shape and color, while neglecting the development of stress-resistant traits, especially cold hardiness [6,7,8]. Breeding methods have predominantly relied on screening wild species and intraspecific hybridization. Consequently, most commercial cultivars originate from a narrow genetic base, leading to reduced genetic diversity, diminished stress tolerance, and pronounced trait imbalance [9]. H. macrophylla cultivars exhibit excellent ornamental traits; however, their limited cold hardiness severely restricts their application in colder regions [10,11]. In contrast, H. arborescens and H. paniculata can endure temperatures as low as −30 °C and demonstrate strong environmental adaptability; however, they exhibit limited flower color variation and possess lower ornamental value [12,13,14].
Interspecific hybridization serves as a viable method for expanding the genetic base and integrating desirable traits from various species [15,16,17,18]. Hybridization involving H. macrophylla with H. arborescens or H. paniculata may produce breakthrough cultivars that integrate rich ornamental traits with strong cold hardiness. Preliminary progress has been reported previously. Several hybrid plants have been produced from crosses involving H. macrophylla as the maternal parent through techniques such as embryo rescue and ovary culture [19,20,21,22]. However, severe interspecific hybridization barriers continue to limit breeding efficiency. All combinations exhibit limited fruit set, poor seed germination, and very low seedling survival, with relatively high compatibility observed only when H. macrophylla was used as the maternal parent. Current research has not adequately clarified the mechanisms underlying these barriers. Feng et al. [23] reported that embryo abortion at the cordate stage primarily contributed to the incompatibility observed between H. macrophylla and H. arborescens. However, their study focused exclusively on crosses in which H. macrophylla served as the maternal parent, omitting reciprocal crosses. Bak and Han [24] evaluated genetic diversity and cross-compatibility among Hydrangea species using SSR markers and controlled pollinations, but direct cytological evidence was not provided. In addition, differences in ploidy can disrupt endosperm balance and impair embryo development [25]. Given that polyploidy is common in H. macrophylla and H. paniculata, variation in ploidy level may further complicate interspecific hybrid compatibility [26,27]. Systematic studies are lacking regarding the types, key developmental stages, and regulatory mechanisms of compatibility barriers in reciprocal crosses between H. macrophylla and H. arborescens, as well as in both direct and reciprocal crosses between H. macrophylla and H. paniculata. This gap has led breeding practices to rely heavily on empirical methods, thereby hindering the development of targeted strategies to address hybridization barriers.
Based on this research background, we conducted systematic direct and reciprocal crosses among H. macrophylla, H. arborescens, and H. paniculata. The objectives of this study were as follows: (1) To assess the occurrence of unidirectional incompatibility in crosses involving H. macrophylla with H. paniculata and H. arborescens, with attention to the potential influence of ploidy differences. (2) To analyze prezygotic and postzygotic barriers in the context of hybridization. For prezygotic barriers, the focus is on pollen germination on the stigma, abnormalities during pollen tube elongation, and whether the tube reaches the ovule. For postzygotic barriers, embryo development was observed using paraffin sections to identify the key periods and features of embryo abortion. (3) To propose practical methods for overcoming these barriers based on their types and underlying mechanisms. The findings of this study provide a theoretical basis and practical guidance for breeding Hydrangea cultivars that integrate excellent ornamental traits with enhanced cold hardiness by clarifying interspecific reproductive barriers.
2. Materials and Methods
2.1. Plant Materials
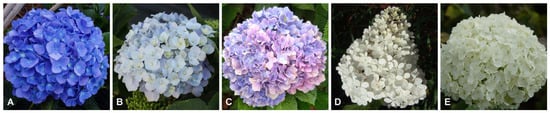
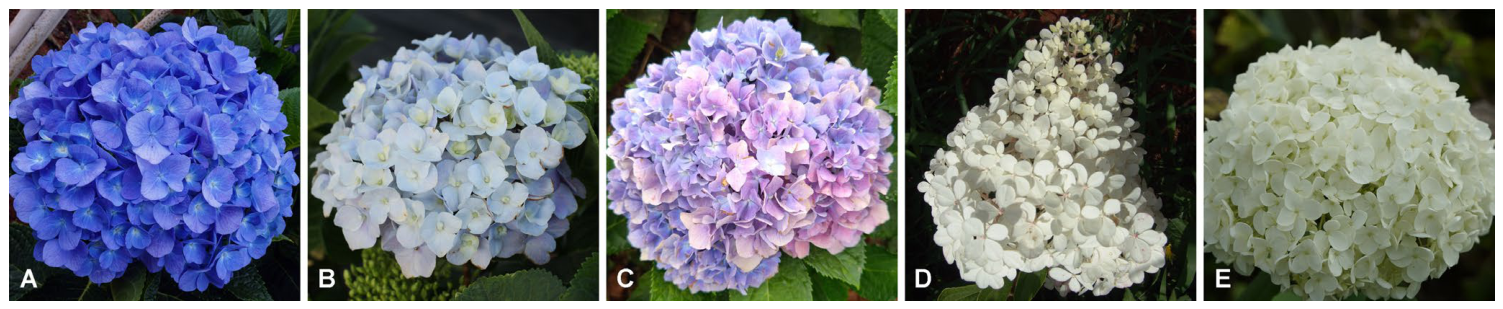
The experimental materials comprised horticultural cultivars of H. macrophylla, H. paniculata, and H. arborescens. The inflorescence morphology of these cultivars is presented in Figure 1. All parent plants were ≥8 years old and had been propagated from cuttings. The specimens were planted in the outdoor setting of the South Tropical Garden at Kunming Yangyueji Horticulture Co., Ltd. (102°58′59″ E, 24°51′32″ N) and managed in accordance with standard horticultural practices.
Figure 1.
Inflorescence morphology of parental plants. (A): H. macrophylla ‘Bodalan’; (B): H. macrophylla ‘Lantian’; (C): H. macrophylla ‘Fanhua’; (D): H. paniculata ‘Strawberry Sundae’; (E): H. arborescens ‘Annabelle’.
2.2. Ploidy Determination
Ploidy levels of the parental cultivars, H. macrophylla ‘Bodalan’, H. paniculata ‘Strawberry Sundae’, and H. arborescens ‘Annabelle’, were estimated by flow cytometry. Three biological replicates were analyzed for each sample. Fresh young leaves were used for nuclear DNA extraction. Tomato (reference genome size 0.9 Gb) [28] was used as an internal standard. Flow cytometric analysis was conducted following the protocol described by Chen et al. [29]. The relative nuclear DNA content of each sample was calculated using the following equation:
Based on previously determined ploidy levels of Hydrangea species using flow cytometry and chromosome counting [29], the ploidy level of each cultivar was estimated by comparing its 2C DNA content with that of the corresponding species:
2.3. Interspecific Hybridization
The experiments were conducted from July to September 2024. The following 12 cross combinations were established:
(1) H. macrophylla ‘Bodalan’ × H. paniculata ‘Strawberry Sundae’;
(2) H. paniculata ‘Strawberry Sundae’ × H. macrophylla ‘Bodalan’;
(3) H. macrophylla ‘Bodalan’ × H. arborescens ‘Annabelle’;
(4) H. arborescens ‘Annabelle’ × H. macrophylla ‘Bodalan’;
(5) H. macrophylla ‘Lantian’ × H. paniculata ‘Strawberry Sundae’;
(6) H. paniculata ‘Strawberry Sundae’ × H. macrophylla ‘Lantian’;
(7) H. macrophylla ‘Lantian’ × H. arborescens ‘Annabelle’;
(8) H. arborescens ‘Annabelle’ × H. macrophylla ‘Lantian’;
(9) H. macrophylla ‘Fanhua’ × H. paniculata ‘Strawberry Sundae’;
(10) H. paniculata ‘Strawberry Sundae’ × H. macrophylla ‘Fanhua’;
(11) H. macrophylla ‘Fanhua’ × H. arborescens ‘Annabelle’;
(12) H. arborescens ‘Annabelle’ × H. macrophylla ‘Fanhua’.
At least ten inflorescences were pollinated in each cross, with each inflorescence containing at least 15 flowers. Pollination was performed according to the method established by Nesi et al. [30]. For the paternal parent, non-decorative flowers were selected for pollen collection, dried, and stored. For the maternal parent, inflorescences containing numerous non-decorative flowers nearing bloom were selected, while decorative flowers and fully opened non-decorative flowers were removed. Hydrangea species are generally considered to exhibit partial or complete self-incompatibility, although self-fertility varies among cultivars and species [13]. Therefore, all maternal flowers were emasculated prior to anthesis to ensure that all recorded seed sets originated from cross-pollination. The petals and stamens of non-decorative flowers were removed using forceps, and the inflorescences were subsequently covered with paper bags to prevent contamination by foreign pollen. Pollination was conducted on the following day between 9:00 and 11:00. Pollen was applied to the stigma using a brush, after which the inflorescences were re-covered with paper bags. Two weeks after pollination, the number of swollen ovaries was recorded, and the paper bags were replaced with breathable mesh bags. Fruits were harvested 70–180 days after pollination (DAP), with fruit set and the number of seeds per fruit recorded before sowing. Seedling emergence was recorded 2–3 months after sowing. The following metrics were calculated:
2.4. Pollen Tube Observation via Fluorescence Microscopy
From the four crosses involving ‘Bodalan’, pistils were collected at 1, 3, 5, 7, 12, 24, 36, 48, 72, and 96 h after pollination (HAP). Pistils were fixed in FAA (70% ethanol: 38% formaldehyde: glacial acetic acid = 90:5:5) for 48 h, transferred to 70% ethanol, and stored at 4 °C. In accordance with the method established by Alexander [26], with minor modifications, the pistils were softened in 4 mol·L−1 NaOH at 60 °C for 3 h, stained with 0.1% aniline blue in the dark for 2 h, and longitudinally sectioned for observation with a fluorescence microscope (DM2500, Leica Microsystems, Wetzlar, Germany). Images were captured and recorded.
2.5. Hybrid Embryo Observation via Paraffin Sectioning
Ovaries were sampled from the four crosses involving ‘Bodalan’ at 0, 1, 3, 5, 7, 10, and 15 DAP, followed by sampling at 5-day intervals until the onset of fruit browning. The outer skin was removed, and the ovaries were fixed in FAA (70% ethanol: 38% formaldehyde: glacial acetic acid = 90:5:5) for at least 48 h. The standard paraffin sectioning method was employed, with sections cut at 8–10 μm, stained with safranin–fast green, and observed with a microscope (CX40-RFL, SOPTOP, Ningbo, China) to document the developmental process and abortion characteristics of hybrid embryos in each cross combination. To quantify the proportion of normal embryos, five ovaries were randomly selected per cross combination at each of the four key embryonic stages (globular, cordate, torpedo, and cotyledonary). The percentage of normal embryos was calculated as the ratio of morphologically normal embryos to the total number of embryos per ovary.
2.6. Statistical Analysis
Microsoft Excel 2016 (Redmond, WA, USA) was used to perform routine statistical analyses on the experimental data. The percentage of normal embryos was subjected to a one-way analysis of variance using IBM SPSS 26.0 (IBM, Inc., Armonk, NY, USA). Results are presented as mean ± standard deviation (n = 5).
3. Results
3.1. Ploidy Determination of Parental Cultivars
Genome size estimation and ploidy analysis were performed for the three parental cultivars. As shown in Table 1, ‘Bodalan’ and ‘Annabelle’ were identified as diploids, whereas ‘Strawberry Sundae’ was determined to be a triploid based on nuclear DNA content analysis.
Table 1.
Genome size estimation and inferred ploidy levels of 3 parental cultivars.
3.2. Fruit Set
Differences were observed among the crossing combinations in the percentages of swollen ovaries, fruit set, and seedling emergence (Table 2). All combinations produced swollen ovaries and fruits. The reciprocal crosses using H. paniculata and H. arborescens as maternal parents exhibited the highest percentages of swollen ovaries, reaching 84.24–96.68% in H. paniculata × H. macrophylla combinations and 97.75–98.72% in H. arborescens × H. macrophylla combinations. However, their fruit set declined more sharply relative to ovary swelling in these combinations, decreasing to 47.00–63.27% and 31.91–43.96%, respectively. In contrast, the direct crosses showed smaller reductions from ovary swelling to fruit set. The fruit set of crosses between H. macrophylla and H. paniculata, in both direct and reciprocal directions, was higher than that of crosses between H. macrophylla and H. arborescens, thereby suggesting that H. macrophylla was more compatible with H. paniculata than with H. arborescens.
Table 2.
Fruit set, seed production, and seedling emergence in 12 crosses.
Regarding seed production, ‘Strawberry Sundae’ × ‘Fanhua’ produced the highest mean number of seeds per fruit (27.62), whereas ‘Annabelle’ × ‘Bodalan’ produced the lowest (2.84). In direct crosses, the mean number of seeds per fruit ranged from 18.00 to 26.18 in H. macrophylla × H. paniculata and from 13.80 to 17.00 in H. macrophylla × H. arborescens.
The percentages of seedling emergence were consistently low across all combinations. Seedling emergence was observed mainly in direct crosses, ranging from 2.96% to 5.61% in H. macrophylla × H. paniculata and from 2.19% to 4.33% in H. macrophylla × H. arborescens. In contrast, reciprocal crosses produced extremely few or no seedlings, with emergence rates of only 0.02–0.03% in H. paniculata × H. macrophylla and 0% in H. arborescens × H. macrophylla. Notably, although reciprocal crosses showed high ovary swelling and fruit set, seed development remained severely limited. Taken together, crosses using H. macrophylla as the maternal parent showed higher seedling emergence than reciprocal crosses, indicating a degree of unilateral compatibility.
3.3. Pollen Tube Growth
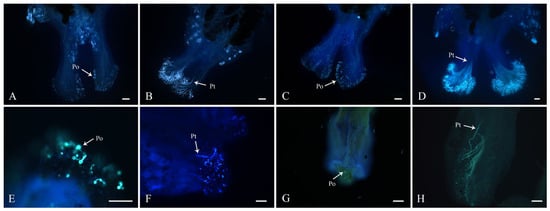
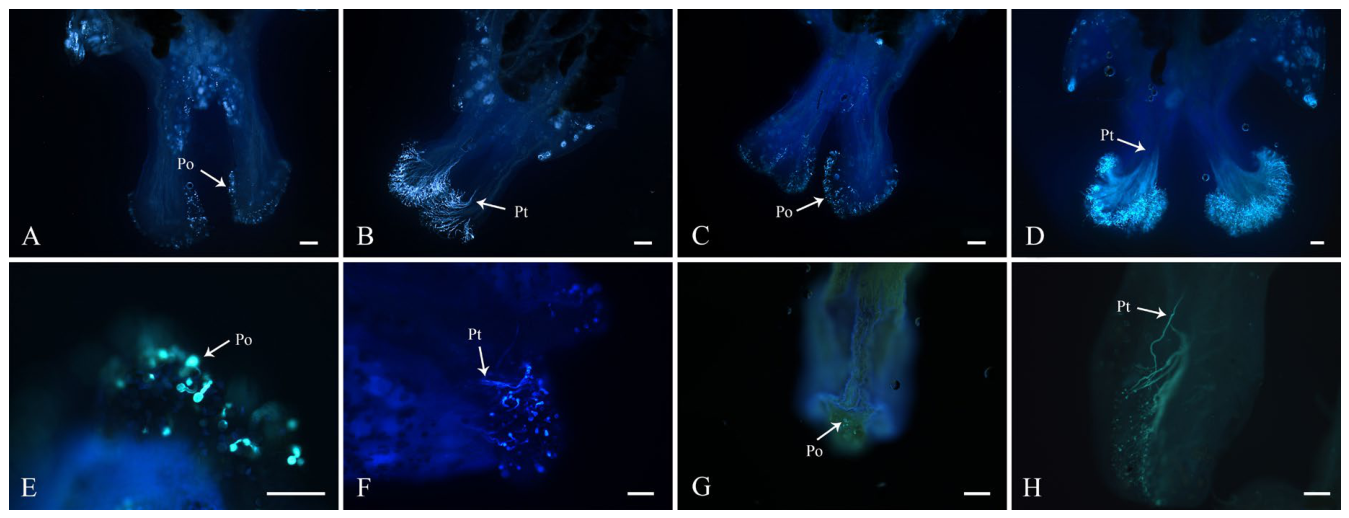
In the four representative crosses involving ‘Bodalan’, all paternal pollen grains adhered to and germinated on the stigmas of the maternal parents, but the timing and extent of germination varied. In the direct crosses, pollen began to germinate at 3–5 h after pollination (HAP), followed by penetration through the papilla cells and downward growth into the style (Figure 2A–D). Compared with ‘Bodalan’ × ‘Strawberry Sundae’, pollen germination in ‘Bodalan’ × ‘Annabelle’ was delayed and less abundant. Notably, pollen of both ‘Strawberry Sundae’ and ‘Annabelle’ exhibited a distinct spiral growth pattern when germinating on the stigmas of ‘Bodalan’; however, this did not reduce germination efficiency. In the reciprocal crosses, pollen germination was strongly inhibited. In ‘Strawberry Sundae’ × ‘Bodalan’, only a small number of pollen grains germinated at 5 HAP, and pollen tube growth was slow, penetrating the stigma only at 24 HAP (Figure 2E,F). In ‘Annabelle’ × ‘Bodalan’, incompatibility was most evident. Very few pollen grains germinated, and only a limited number of pollen tubes penetrated the stigmatic tissue (Figure 2G,H).
Figure 2.
Pollen germination on stigmas after pollination in four crosses. (A): ‘Bodalan’ × ‘Strawberry Sundae’ at 3 HAP; (B): ‘Bodalan’ × ‘Strawberry Sundae’ at 5 HAP; (C): ‘Bodalan’ × ‘Annabelle’ at 5 HAP; (D): ‘Bodalan’ × ‘Annabelle’ at 7 HAP; (E): ‘Strawberry Sundae’ × ‘Bodalan’ at 5 HAP; (F): ‘Strawberry Sundae’ × ‘Bodalan’ at 24 HAP; (G): ‘Annabelle’ × ‘Bodalan’ at 3 HAP; (H): ‘Annabelle’ × ‘Bodalan’ at 7 HAP. Po: Pollen; Pt: Pollen tube. Scale bar = 100 μm.
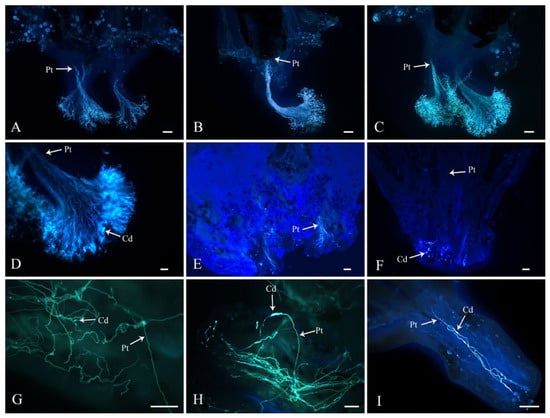
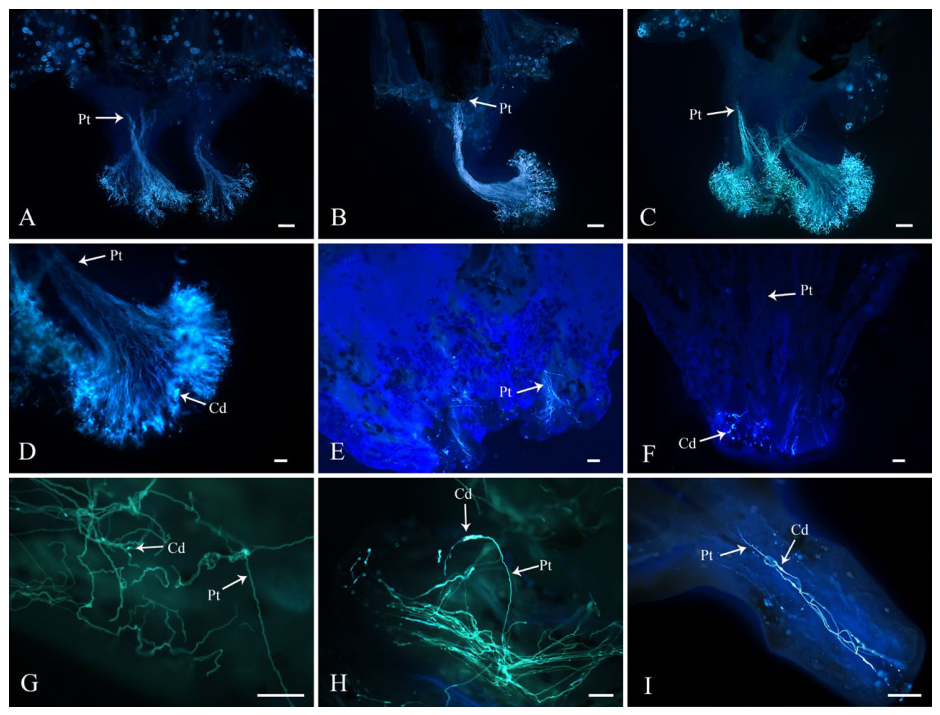
After entering the style, pollen tubes from all four combinations exhibited both normal and abnormal growth. In the direct crosses, pollen tubes in ‘Bodalan’ × ‘Strawberry Sundae’ elongated continuously within the style and reached the style base at 36 HAP (Figure 3A,B). In ‘Bodalan’ × ‘Annabelle’, pollen tube growth followed a similar pattern but progressed more slowly (Figure 3C,D). During elongation in both direct crosses, some pollen tubes exhibited callose deposition, coiling, or lateral growth. In contrast, pollen tube growth was more restricted in the reciprocal crosses. Tubes showed twisting, severe callose deposition, and coiling, with very few reaching the style base even by 24–72 HAP (Figure 3E–I).
Figure 3.
Pollen tube elongation in styles in four crosses. (A): ‘Bodalan’ × ‘Strawberry Sundae’ at 12 HAP; (B): ‘Bodalan’ × ‘Strawberry Sundae’ at 36 HAP; (C): ‘Bodalan’ × ‘Annabelle’ at 12 HAP; (D): ‘Bodalan’ × ‘Annabelle’ at 24 HAP; (E): ‘Strawberry Sundae’ × ‘Bodalan’ at 48 HAP; (F–H): ‘Strawberry Sundae’ × ‘Bodalan’ at 72 HAP; (I): ‘Annabelle’ × ‘Bodalan’ at 24 HAP. Pt: Pollen tube; Cd: Callose deposition. Scale bar = 100 μm.
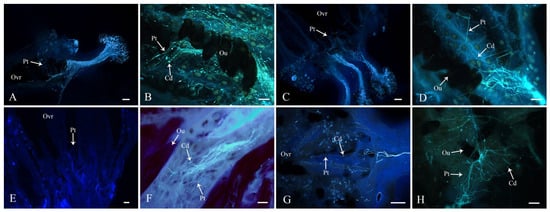
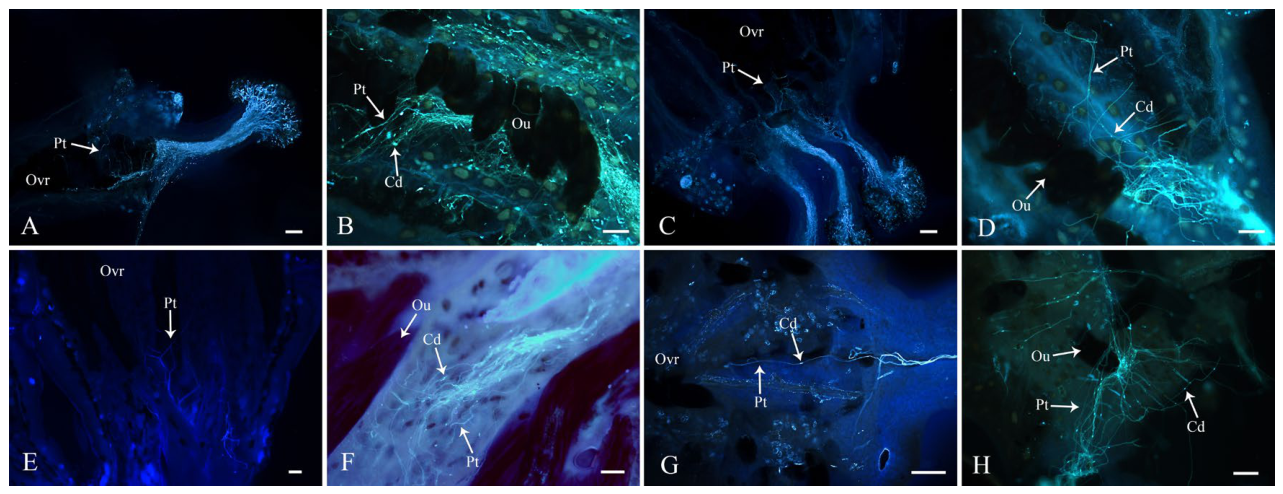
Once the pollen tubes entered the ovary, their behavior varied markedly among combinations. Abnormalities, such as swelling or bursting at tube tips, were frequently observed. In direct crosses, most tubes successfully reached ovules by 72–96 HAP, despite some breakage or callose deposition (Figure 4A–D). In reciprocal crosses, very few pollen tubes entered the ovary by 48–96 HAP, and even at 96 HAP, the number of tubes reaching ovules remained low (Figure 4H).
Figure 4.
Pollen tube entry into ovaries in four crosses. Note: (A,B): ‘Bodalan’ × ‘Strawberry Sundae’ at 72 HAP; (C): ‘Bodalan’ × ‘Annabelle’ at 72 HAP; (D): ‘Bodalan’ × ‘Annabelle’ at 96 HAP; (E,F): ‘Strawberry Sundae’ × ‘Bodalan’ at 96 HAP; (G): ‘Annabelle’ × ‘Bodalan’ at 48 HAP; (H): ‘Annabelle’ × ‘Bodalan’ at 96 HAP. Pt: Pollen tube; Cd: Callose deposition; Ovr: Ovary; Ou: Ovule. Scale bar = 100 μm.
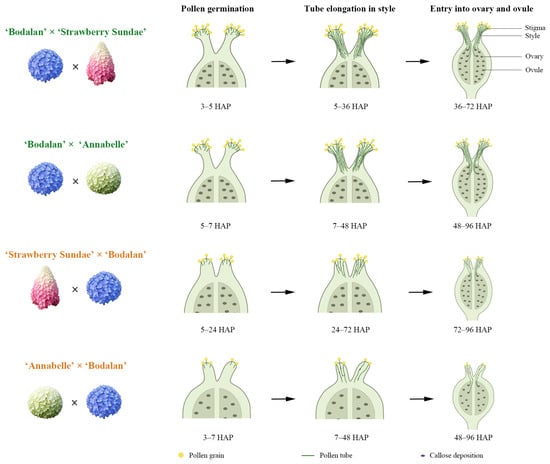
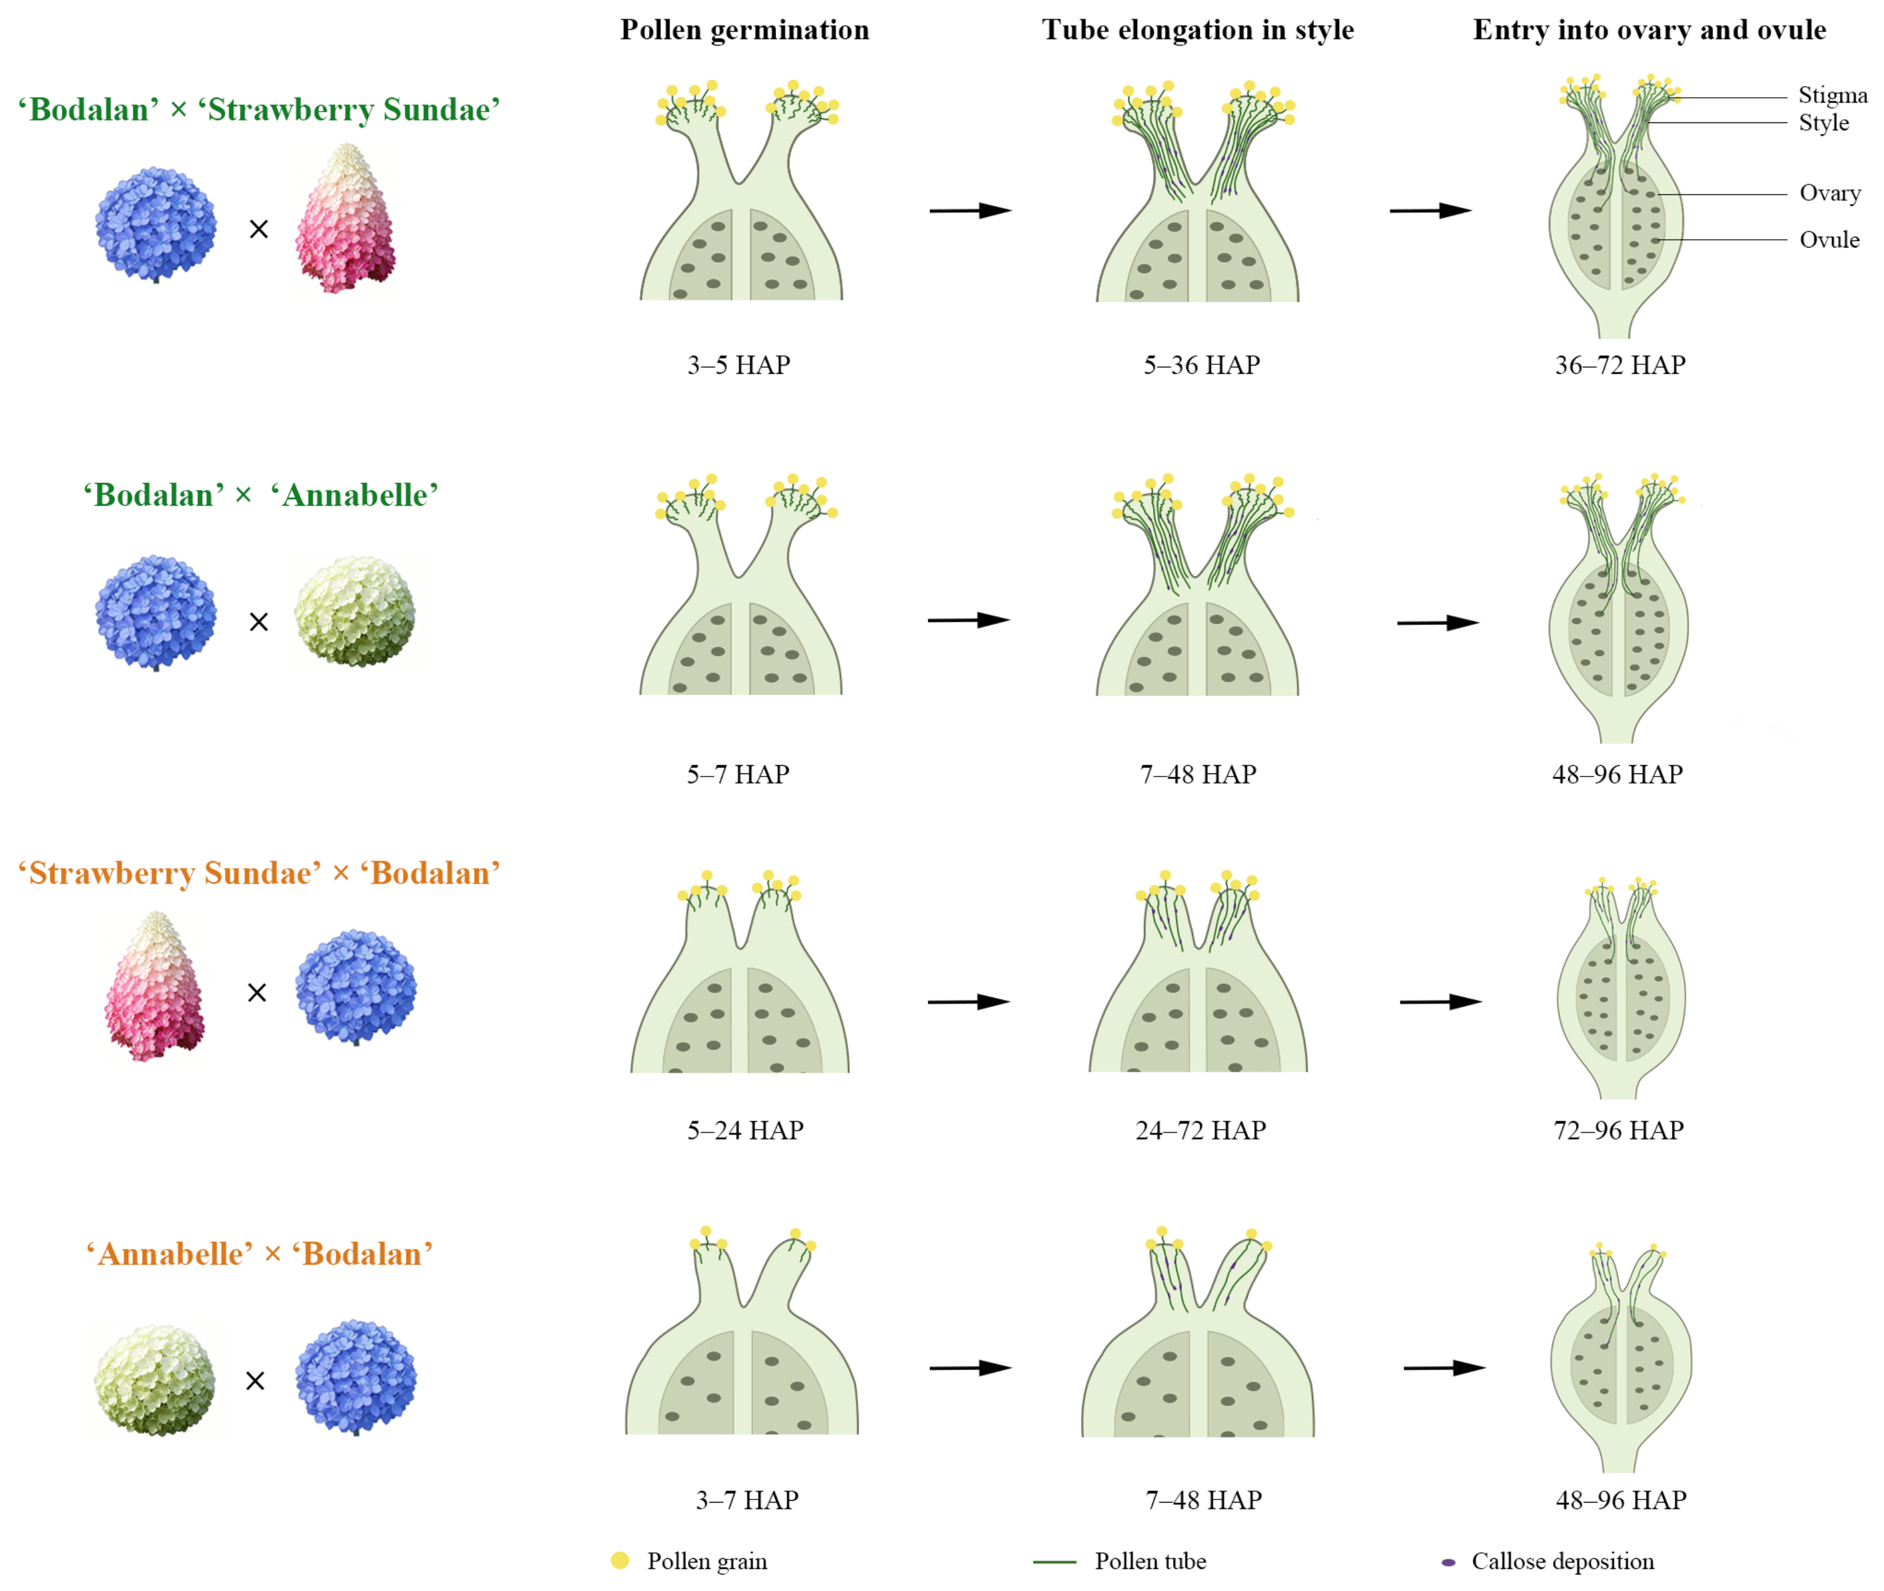
In summary, all four combinations showed prezygotic barriers, but their severities varied (Figure 5). The direct crosses exhibited mild barriers that were not the main cause of incompatibility. Although spiral growth and localized callose deposition occurred during pollen germination and tube elongation, many pollen tubes still reached the ovules. In contrast, the prezygotic barriers were severe in the reciprocal crosses. These crosses exhibited reduced pollen germination, delayed germination, and marked abnormalities during pollen tube growth, resulting in few pollen tubes reaching the ovules.
Figure 5.
Schematic representation of pollen germination and pollen tube growth in four crosses.
3.4. Embryo Development and Embryo Abortion
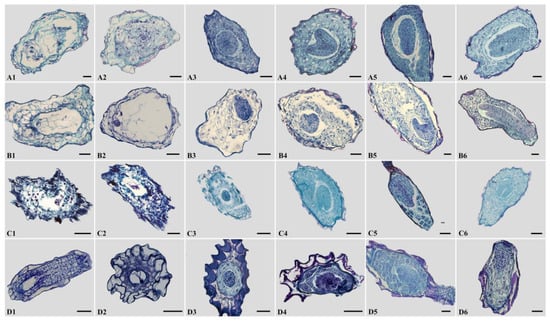
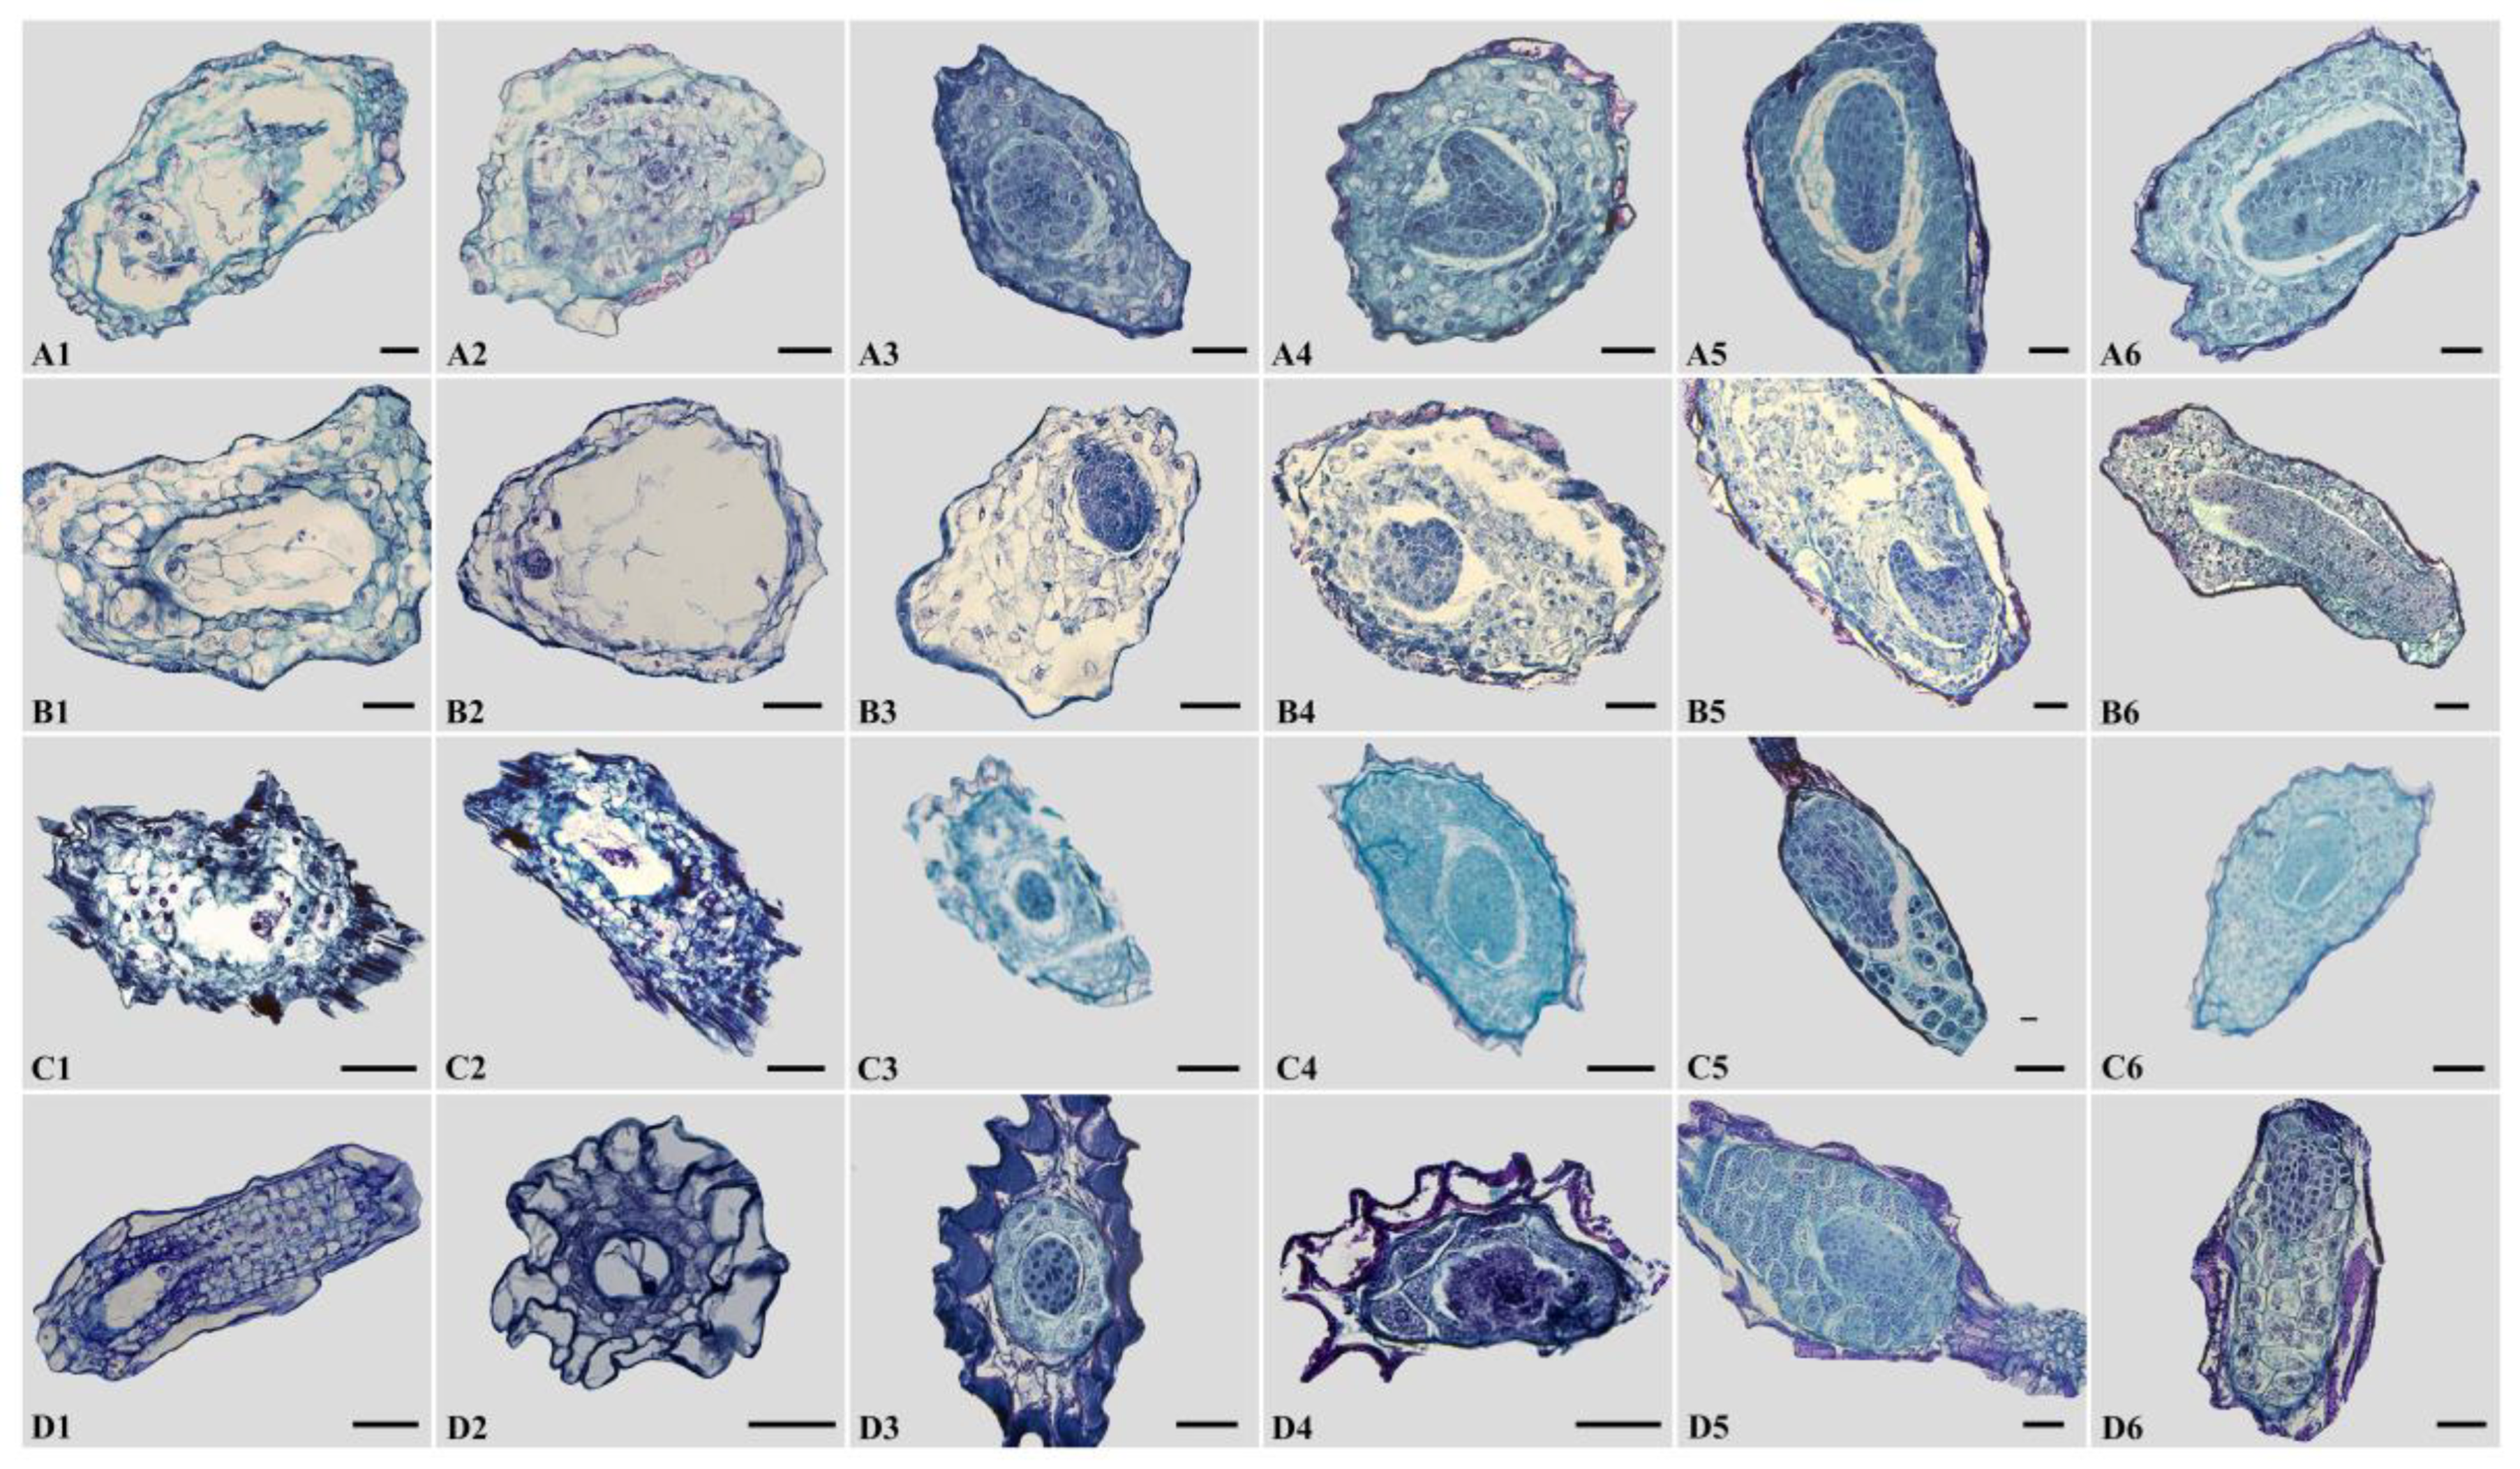
Normal embryo development was observed in the four selected cross combinations, although the developmental pace differed between direct and reciprocal crosses (Figure 5). In the direct crosses, embryo development proceeded relatively slowly, although slight differences were observed between combinations. In ‘Bodalan’ × ‘Strawberry Sundae’, free-nuclear endosperm and enlarged embryo sacs were observed at 25 DAP (Figure 6A1). The proembryo formed at 35 DAP, characterized by initial cell divisions of densely cytoplasmic cells (Figure 6A2). The globular embryo stage, consisting of isodiametric and actively dividing cells, was reached at 55 DAP (Figure 6A3). This was followed by the cordate stage at 70 DAP, marked by the emergence of cotyledon primordia and establishment of bilateral symmetry (Figure 6A4), and torpedo at 80 DAP, characterized by elongation of the embryo axis (Figure 6A5). A mature embryo with symmetrical cotyledons was observed at 115 DAP (Figure 6A6). In the cross with ‘Annabelle’, a similar developmental sequence was observed. However, fertilization-related events occurred slightly earlier, with sperm cells adhering to the secondary polar nuclei at 20 DAP (Figure 6B1). The proembryo was observed at 35 DAP (Figure 6B2), after which the embryo developed sequentially through the globular at 50 DAP (Figure 6B3), cordate at 55 DAP (Figure 6B4), and torpedo at 70 DAP (Figure 6B5), ultimately reaching maturity at 115 DAP (Figure 6B6), although the overall developmental pace remained relatively slow. Reciprocal crosses exhibited a faster developmental pace. In ‘Strawberry Sundae’ × ‘Bodalan’, polar nuclear fusion occurred at 3 DAP (Figure 6C1), followed by sperm cells adhering to the secondary polar nuclei (Figure 6C2). The globular embryo was observed at 25 DAP, showing a spherical structure of actively dividing cells (Figure 6C3). The embryo quickly developed into the cordate stage at 30 DAP (Figure 6C4), with visible cotyledon primordia, and then into the torpedo stage at 40 DAP, marked by elongation of the embryo axis (Figure 6C5). The cotyledon embryo with distinct radicle, plumule, and cotyledons formed at 75 DAP (Figure 6C6). In ‘Annabelle’ × ‘Bodalan’, polar nuclear fusion occurred at 7 DAP (Figure 6D1). The zygote remained undivided until 20 DAP (Figure 6D2). After division began, embryo development accelerated. The globular embryo was observed at 40 DAP (Figure 6D3). Subsequently, it entered the cordate stage at 45 DAP (Figure 6D4) and torpedo stage at 50 DAP (Figure 6D5). A mature embryo with radicle, plumule, and cotyledons was observed at 60 DAP (Figure 6D6).
Figure 6.
Fertilization and embryo development process in four crosses. (A1–A6): ‘Bodalan’ × ‘Strawberry Sundae’; (B1–B6): ‘Bodalan’ × ‘Annabelle’; (C1–C6): ‘Strawberry Sundae’ × ‘Bodalan’; (D1–D6): ‘Annabelle’ × ‘Bodalan’. Scale bar = 50 μm.
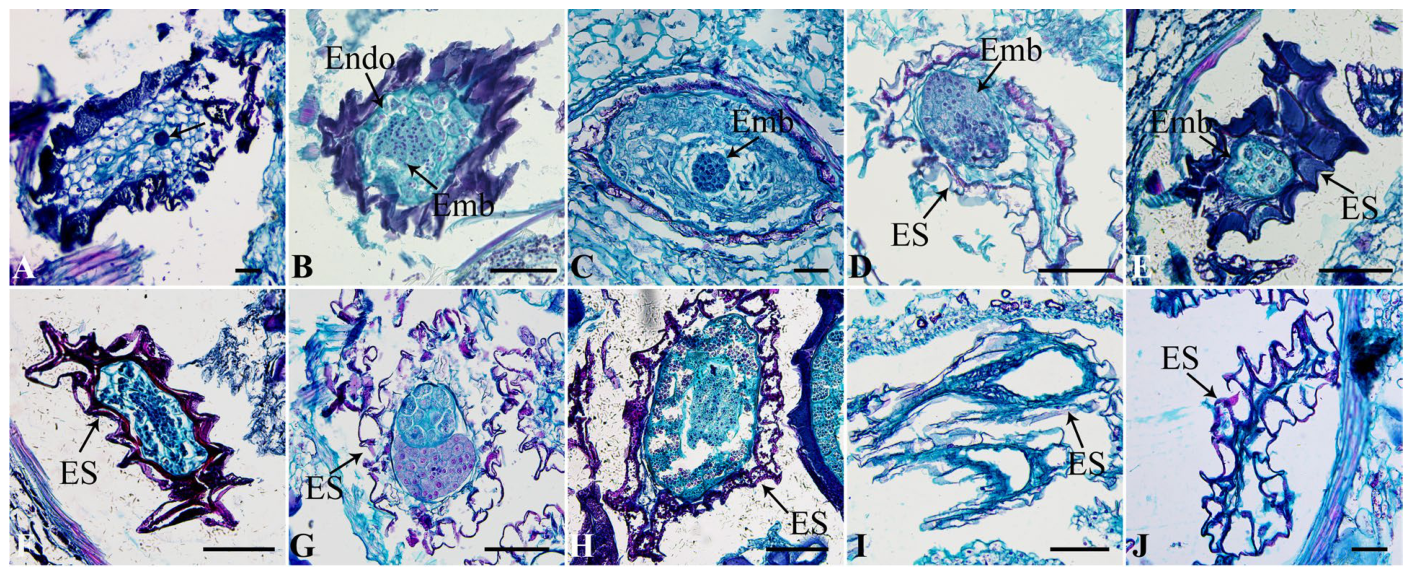
Paraffin section observations revealed four types of embryo abortion, which differed in abortion characteristics, cross combinations, and developmental stages: I. Embryo-type abortion: Endosperm development was normal, whereas the zygote or embryo showed developmental abnormalities. The zygote either failed to divide (Figure 7A) or showed abnormal division patterns. In some cases, embryos exhibited clear morphological deformities, such as irregular shape and loss of structural symmetry (Figure 7B), or remained arrested at an early stage, such as the globular stage, without further differentiation (Figure 7C). This type of abortion was observed from the torpedo to cotyledonary stages and only in reciprocal crosses. II. Endosperm-type abortion: Endosperm development was severely impaired, characterized by a marked reduction in endosperm volume or complete degeneration. Embryo development was delayed or weak due to an insufficient nutrient supply, and mild malformations were often observed; however, the basic structure remained recognizable (Figure 7D). This was the main type of embryo abortion in direct crosses and occurred mainly during the globular to cordate embryo stages. III. Complete abortion: Both embryonic and endosperm development failed completely. Typical features included severe tissue deformation, disordered cell arrangement, structural identity loss, or cellular organization collapse. Four subtypes were observed: (1) severe endosperm degeneration with a malformed embryo or early developmental arrest with limited cell division (Figure 7E); (2) retention of a small amount of endosperm with a shrunken and malformed embryo (Figure 7F); (3) embryo and endosperm tissues forming separate, disorganized clusters without clear structural identity (Figure 7G); and (4) progressive disintegration of embryo sac tissues, with collapse of cellular organization (Figure 7H). This type of abortion occurred mainly at the middle and late stages of embryo development (globular to cotyledonary) and was frequent in reciprocal crosses but rare in direct crosses. IV. Cavity and atrophy type: No recognizable embryo or endosperm structures was present within the embryo sac. The embryo sac either appeared as an empty cavity (Figure 7I) or showed overall atrophy (Figure 7J). This type was likely caused by unsuccessful double fertilization or rapid degeneration of the zygote and primary endosperm nucleus after fertilization. It occurred at all developmental stages in all four cross combinations but was more frequent in reciprocal crosses. Clear differences in both the type and severity of embryo abortion were observed among the cross combinations and were strongly associated with the crossing direction. In direct crosses, embryo abortion was mainly represented by Types II and IV, and the overall severity was relatively mild. In contrast, reciprocal crosses were dominated by Types I, III, and IV, with Type III being the most frequent and severe.
Figure 7.
Embryo abortion phenomena. (A): ‘Strawberry Sundae’ × ‘‘Bodalan’ at 70 DAP, zygote undivided; the arrow indicates the undivided zygote; (B): ‘Annabelle’ × ‘Bodalan’ at 60 DAP, embryo malformed; (C): ‘Strawberry Sundae’ × ‘Bodalan’ at 70 DAP, embryo arrested at globular stage; (D): ‘Bodalan’ × ‘Annabelle’ at 70 DAP, severe endosperm degeneration; (E): ‘Annabelle’ × ‘Bodalan’ at 60 DAP, severe endosperm degeneration with reduced embryonic cell division; (F): ‘Annabelle’ × ‘Bodalan’ at 80 DAP, embryo sac atrophied; (G): ‘Strawberry Sundae’ × ‘Bodalan’ at 50 DAP, embryo and endosperm developed as separate, disorganized cell clusters; (H): ‘Annabelle’ × ‘Bodalan’ at 80 DAP, disintegrated embryo sac tissues and cellular wall collapse; (I): ‘Strawberry Sundae’ × ‘Bodalan’ at 50 DAP: empty embryo sac; (J): ‘Strawberry Sundae’ × ‘Bodalan’ at 50 DAP: atrophied embryo sac with no contents. Emb: embryo. Endo: endosperm. ES: embryo sac. Scale bar = 100 μm.
To quantitatively assess the severity of embryo abortion, the proportion of normal embryos at different developmental stages was analyzed for each combination (Table 3). Direct crosses with ‘Bodalan’ as the maternal parent consistently showed higher proportions of normal embryos at all stages than those observed for reciprocal crosses. Among them, ‘Bodalan’ × ‘Strawberry Sundae’ had the highest proportion of normal embryos, followed by ‘Bodalan’ × ‘Annabelle’. Reciprocal crosses showed extremely low proportions of normal embryos, dropping below 10% at the globular embryo stage and approaching zero at later stages. ‘Annabelle’ × ‘Bodalan’ had the lowest values, decreasing to 1.46% at the cordate stage and only reaching 0.63–0.87% after the torpedo stage. These results are consistent with the severe embryo abortion observed morphologically in reciprocal crosses. In all four crosses, the proportion of normal embryos declined progressively as embryonic development advanced; however, the rate of decline differed among the combinations. In ‘Bodalan’ × ‘Strawberry Sundae’, the most rapid decrease occurred from the torpedo to cotyledonary stages. In ‘Bodalan’ × ‘Annabelle’, the largest decline occurred from the cordate to torpedo stages, with a reduction of 9.21%. The decline in ‘Strawberry Sundae’ × ‘Bodalan’ was relatively gradual across all stages. ‘Annabelle’ × ‘Bodalan’ showed a sharp decrease of 7.3% from the globular to cordate stages.
Table 3.
Percentage of normal embryos at four dates after pollination in four crosses.
4. Discussion
4.1. Interspecific Cross-Compatibility Among H. macrophylla, H. paniculata, and H. arborescens
This study revealed pronounced unilateral incompatibility in interspecific crosses involving H. macrophylla with both H. paniculata and H. arborescens. Direct crosses using H. macrophylla as the maternal parent produced a proportion of normal embryos and a limited number of seedlings, with emergence rates between 2.19% and 5.61%. In contrast, reciprocal crosses were largely unsuccessful. Although percentages of swollen ovaries exceeded 84%, seed development was severely restricted, leading to extremely low seedling emergence rates (0–0.03%). This finding aligns with previous reports indicating that successful progeny are rarely obtained when H. paniculata or H. arborescens serve as the maternal parent. In contrast, employing H. macrophylla as the maternal parent substantially improves hybrid fertility [13,20]. Therefore, H. macrophylla is recommended as the preferred maternal parent for interspecific hybridization with H. paniculata or H. arborescens. Importantly, ovary swelling may not necessarily reflect successful fertilization, as it can also result from pollination-induced hormonal responses [31]. Therefore, fruit set and seeding emergence provide more reliable indicators of compatibility. Regardless of the crossing direction, the combinations of H. macrophylla and H. paniculata generally exhibited higher fruit set, greater seed numbers per fruit, and higher proportions of normal embryos than the combinations of H. macrophylla and H. arborescens. This pattern may be attributed to geographic origins and genetic relationships. H. macrophylla is native to China and Japan, with its distribution overlapping that of H. paniculata, which ranges from East Asia to eastern North America [32,33,34]. In contrast, H. arborescens is native to North America, where long-term geographic isolation promotes genetic divergence, thereby enhancing reproductive isolation from other groups [1,35]. Molecular phylogenetic studies have indicated that H. macrophylla and H. paniculata are closely related lineages within the genus, sharing high similarity in their nuclear and chloroplast genomes, whereas H. arborescens is more distantly related [36,37]. Genetic relatedness serves as the key basis for parental selection in hybrid breeding. Research indicates that successful hybridization between two Hydrangea species or closely related genera becomes challenging when the genetic distance coefficient (GDC) exceeds 0.01385 [38]. In these cases, intermediate species capable of crossing with both parents may facilitate the resolution of reproductive isolation [39,40,41].
Crosses between diploid ‘Bodalan’ and triploid ‘Strawberry Sundae’ exhibited higher compatibility than those between diploid ‘Bodalan’ and diploid ‘Annabelle’, regardless of crossing direction. This observation contrasts with the commonly reported positive relationship between parental ploidy similarity and hybridization success [25,42], suggesting that genetic distance may play a more dominant role than ploidy differences in determining interspecific compatibility in Hydrangea. Alexander et al. reported that H. macrophylla exhibits a relatively high tolerance to aneuploidy, and that using triploids as maternal parents may improve hybridization success [26]. However, in this study, crosses using the triploid ‘Strawberry Sundae’ as the maternal parent did not outperform those using ‘Bodalan’, implying that the mechanisms underlying compatibility may differ between interspecific and intraspecific hybridization.
4.2. Prezygotic Barriers and Their Possible Alleviation
Prezygotic barriers in distant hybridization typically include reduced pollen germination, obstruction of pollen tube elongation, and failure of pollen tubes to reach the embryo sac [43,44,45]. During normal pollen germination, papilla cells secrete callose to protect maternal tissues. However, in distant hybridization, low compatibility often leads to excessive callose deposition, thereby resulting in twisted, swollen, or branched pollen tubes that impede fertilization [46,47,48,49]. In this study, the prezygotic barriers in direct crosses were relatively mild. Although the pollen tubes displayed spiral growth and localized callose deposition, most tubes successfully reached the ovules within a normal time frame and completed fertilization. In contrast, reciprocal crosses exhibited severe prezygotic barriers. The stylar environment of ‘Strawberry Sundae’ or ‘Annabelle’ strongly inhibited ‘Bodalan’ pollen. This inhibition was characterized by delayed and reduced pollen germination, abnormal pollen tube morphology, and pronounced tube elongation obstruction. Consequently, only a few pollen tubes successfully reached the ovules. Temperature and humidity modulate pollen germination and tube growth in many woody plants. Suboptimal temperatures can reduce pollen viability, inhibit pollen tube growth, and impair fertilization [50]. In crosses of Gossypium hirsutum, relative humidity influences pollen tube growth length [51]. In this study, all crosses were conducted under comparable conditions (20–30 °C, 60–80% RH), suggesting that environmental variation is unlikely to account for the observed direction-dependent differences. Molecular studies have shown that in Arabidopsis, the RALF4/19 signaling pathway regulates pollen tube integrity and modulates the pace and direction of growth through calcium signaling [52]. The observed inhibition of pollen tube growth may be associated with a calcium gradient imbalance at the pollen tube tip. Moreover, reciprocal crosses may encounter additional challenges in the recognition between pollen wall proteins and stigma cells. Lan et al. [53] proposed a lock-and-key model for Arabidopsis interspecific and intergeneric crosses, in which FER/ANJ receptor complexes on stigma papilla cells, in conjunction with autocrine sRALF peptides, constitute the “lock,” while pRALF peptides secreted by compatible pollen act as the “key.” Only pollen from the maternal species or its close relatives can activate this system and achieve fertilization. A similar mechanism may operate in Hydrangea interspecific crosses. Applying synthetic pollen-derived recognition molecules to stigmas or using mixed compatible pollen during pollination may help improve the pollen tube penetration efficiency in reciprocal crosses [54,55,56].
4.3. Postzygotic Barriers and Their Potential Mitigation
Postzygotic embryo abortion was determined to be the primary cause of failed interspecific hybridization involving H. macrophylla with H. paniculata or H. arborescens. This study systematically classified embryo abortion types and revealed clear distinctions between direct and reciprocal crosses. In direct crosses, abortion was dominated by Type II (endosperm-type abortion). Poor endosperm development or early endosperm degeneration disrupted nutrient supply, resulting in embryo abortion mainly during the transition from the globular to cordate embryo stages. This pattern is consistent with that reported by Feng et al. [23]. The endosperm balance number (EBN) is closely associated with parental ploidy, and hybridizations between species with mismatched EBN values result in endosperm abortions [57,58]. Moreover, metabolic disruption contributes to embryo abortion in Hydrangea interspecific hybrids. At the cordate stage of hybrid embryos, the upregulation of the key shikimate pathway gene HmDAHPS induces excessive salicylic acid accumulation, ultimately triggering embryo abortion [23]. Therefore, parental combinations with compatible ploidy levels and EBN values should be preferentially selected. Environmental stress during early seed development, such as elevated temperatures or water deficit, can exacerbate embryo abortion by disrupting carbohydrate metabolism and hormonal balance [50,59]. Therefore, maintaining appropriate environmental conditions is important for ensuring normal embryo development during interspecific hybridization. Embryo rescue should be performed during early embryo stagnation, and supplementation with SA synthesis inhibitors in the culture medium may help bypass endosperm developmental barriers. The success of embryo rescue depends on the accurate timing of embryo collection [60,61]. Based on the present observations, the optimal collection time for embryo rescue in ‘Bodalan’ is approximately 50–60DAP, corresponding to the globular to cordate embryo stages. Reciprocal crosses demonstrated earlier and more severe postzygotic barriers. These crosses were dominated by Type I (embryo-type abortion) and Type III (complete abortion), alongside a high frequency of Type IV (cavity- and atrophy-type abortion) throughout development. This indicates that when H. macrophylla serves as the paternal parent, many ovules fail to complete fertilization or abort shortly thereafter, while some fertilized embryos experience severe developmental disruption and eventual degeneration. As reciprocal crosses face both prezygotic and postzygotic barriers, prioritizing the alleviation of prezygotic barriers is essential for establishing conditions conducive to normal embryo development.
While this study clarifies key reproductive barriers in Hydrangea interspecific crosses, several limitations should be acknowledged. The hybridization experiments were conducted using a limited number of cultivars representing H. paniculata and H. arborescens, which may not fully reflect cross-compatibility variation among H. macrophylla, H. paniculata, and H. arborescens. These experiments were performed within the same flowering period under similar field conditions, which likely minimized environmental variation. However, their potential effects on reproductive success cannot be completely excluded. In addition, the present analyses were based primarily on morphological and histological evidence; consequently, the underlying molecular mechanisms were not directly investigated. Moreover, although several breeding-oriented strategies were proposed based on the observed patterns, their effectiveness remains to be validated through practical breeding trials.
5. Conclusions
In summary, this study revealed unilateral incompatibility in distant crosses involving H. macrophylla and H. paniculata and H. arborescens. In direct crosses, postzygotic endosperm-type abortion served as the primary limiting factor, whereas reciprocal crosses faced restrictions from severe prezygotic pollen tube inhibition and early postzygotic embryo collapse. Furthermore, cross-compatibility was closely related to phylogenetic distance, with genetically similar species (H. macrophylla and H. paniculata) demonstrating higher compatibility, whereas the effect of ploidy was weaker than that of genetic distance. Based on these findings, the following breeding strategies are proposed: (1) Parent selection. H. macrophylla should be prioritized as maternal parents in crosses with H. paniculata or H. arborescens. For genetically distant combinations (e.g., H. macrophylla × H. arborescens), intermediate bridge species may help overcome reproductive isolation. (2) Targeted barrier-overcoming measures: For direct crosses, priority should be given to postzygotic barriers by timely embryo rescue at the globular to cordate stages and optimization of culture media. For reciprocal crosses, efforts should focus on prezygotic barriers via pollen pretreatment, stigma modification, or mixed-compatible pollen pollination to enhance pollen germination and tube growth. This study identified the types, critical stages, and species-specific features of interspecific hybridization barriers in Hydrangea, providing a theoretical basis for parent selection and the technical optimization of breeding programs. However, further studies are needed to validate these strategies.
Author Contributions
H.L. and S.C. designed the study and drafted the manuscript. H.L., S.C. and M.S. performed the experiments and statistical analysis. H.D. and L.T. prepared samples and assisted with experiments. Y.Y. and Z.Y. provided technical assistance with experiments. M.C. supervised the study and revised the manuscript. All authors reviewed the manuscript. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Shanxi Transportation Greening Landscape Engineering Plant Configuration and Cultivation Technology Research Project (SXLQ-LHGS-2-KYLX-3-001-2024) and the Hangzhou Biodiversity Conservation and Assessment Project (2023HXSYL05).
Data Availability Statement
All the data used in this research are presented completely herein.
Conflicts of Interest
Authors Yuyong Yang and Zenghua Yang were employed by the company Kunming Yangyueji Horticulture Co., Ltd. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest. The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results.
References
- Wei, Z.F. A Revision of the Genus Hydrangea in China. Guihaia 1994, 14, 21. [Google Scholar]
- Kitamura, Y.; Fudano, T.; Kawanishi, Y. Relation Between Floral Initiations on Apical Buds of Basal Shoots After the Autumn and Cultivar Differences in Unseasonal Flowering of Hydrangea. Hortic. J. 2020, 89, 488–495. [Google Scholar] [CrossRef] [Scilit]
- Mcclintock, E. A Monograph of the Genus Hydrangea. Proc. Calif. Acad. Sci. 1957, 29, 147–256. [Google Scholar]
- Venturieri, G.; Nesi, B.; Lazzereschi, S.; Pecchioli, S.; Burchi, G. Development of Pollination and in Vitro Germination Techniques to Improve the Hybridization in Hydrangea spp. Adv. Hortic. Sci. 2017, 31, 45–51. [Google Scholar] [CrossRef] [Scilit]
- Sevilleno, S.; Tran, M.; Yi, J.; Park, H.-W.; Hwang, Y. A Review of the Cytogenetic Studies in Hydrangea. Flower Res. J. 2025, 33, 1–11. [Google Scholar] [CrossRef] [Scilit]
- Kitamura, Y.; Hattori, T.; Mogami, K.; Fudano, T.; Uehara, M. Selection of Hydrangea (Hydrangea spp.) Cultivars with High Potential for Unseasonable Flower Bud Production in Japan. Hortic. J. 2018, 87, 532–540. [Google Scholar] [CrossRef] [Scilit]
- Wu, X.; Alexander, L. Genetic Diversity and Population Structure Analysis of Bigleaf Hydrangea Using Genotyping-by-Sequencing. J. Am. Soc. Hortic. Sci. 2019, 144, 257–263. [Google Scholar] [CrossRef] [Scilit]
- Xu, T.; Li, A.; Cui, Y.; Li, Z.; Zhou, M.; Xiong, H.; Liu, G.; Yang, Z.; Yang, Z.; Tong, Y.; et al. Analysis and Comprehensive Evaluation of the Phenotypic Diversity of Hydrangea Germplasm Resources. Res. Sq. 2025. [Google Scholar] [CrossRef] [Scilit]
- Wiedemann, M.; Meinl, K.; Samain, M.-S.; Klocke, E.; Abel, S.; Wanke, S. Intergeneric Hybrids Between Species of Hydrangea and Dichroa-Their Germination In Vivo and In Vitro and Molecular Verification by RAPD Analysis. In Acta Horticulturae 1087: XXV International EUCARPIA Symposium Section Ornamentals: Crossing Borders; International Society for Horticultural Science (ISHS): Leuven, Belgium, 2015; Volume 1087, pp. 333–338. [Google Scholar] [CrossRef] [Scilit]
- Pagter, M.; Liu, F.; Jensen, C.R.; Petersen, K.K. Effects of Chilling Temperatures and Short Photoperiod on PSII Function, Sugar Concentrations and Xylem Sap ABA Concentrations in Two Hydrangea Species. Plant Sci. 2008, 175, 547–555. [Google Scholar] [CrossRef] [Scilit]
- Chen, H.J.; Yan, Z.F.; Qi, X.Y.; Chen, S.S.; Feng, J.; Jin, Y.Y.; Miao, Y.H.; Deng, Y.M. Evaluation of cold tolerance and screening of main indicators in different Hydrangea cultivars. J. Plant Resour. Environ. 2024, 33, 41–49. [Google Scholar]
- Dirr, M.A. Manual of Woody Landscape Plants; Stipes Publishing Company: Champaign, IL, USA, 1998. [Google Scholar]
- Reed, S.M. Compatibility Studies in Hydrangea. J. Environ. Hortic. 2000, 18, 29–33. [Google Scholar] [CrossRef] [Scilit]
- Xue, C.; Wen, Y.; Sheng, S.; Gao, Y.; Zhang, Y.; Chen, T.; Peng, J.; Cao, S. Hormonal Regulation and Transcriptomic Insights into Flower Development in Hydrangea Paniculata ‘Vanilla Strawberry’. Plants 2024, 13, 486. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Singh, D.P.; Singh, A.K.; Singh, A. Plant Breeding and Cultivar Development, 1st ed.; Academic Press: London, UK, 2021. [Google Scholar]
- Kopecký, D.; Martín, A.; Smýkal, P. Interspecific Hybridization and Plant Breeding: From Historical Retrospective through Work of Mendel to Current Crops. Czech J. Genet. Plant Breed. 2022, 58, 113–126. [Google Scholar] [CrossRef] [Scilit]
- García, A.V.; Chalup, L.; Seijo, J.G. Toward the Development of a Cross-compatibility Framework to Enhance the Utilization of Peanut CWRs. Crop Sci. 2024, 64, 2961–2976. [Google Scholar] [CrossRef] [Scilit]
- Shrestha, A.; Stephens, C.J.; Angeles-Shim, R.B. Taming Wild Genomes: Perspectives on Mechanisms Governing Differential Introgression in Exotic Rice Germplasm and Their Applications in Breeding. Front. Plant Sci. 2025, 16, 1489244. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kudo, N.; Niimi, Y. Production of Interspecific Hybrids between Hydrangea macrophylla f. Hortensia (Lam.) Rehd. and H. arborescens L. J. Jpn. Soc. Hortic. Sci. 1999, 68, 428–439. [Google Scholar] [CrossRef] [Scilit]
- Reed, S.M.; Riedel, G.L.; Pooler, M.R. Verification and Establishment of Hydrangea macrophylla ‘Kardinal’ x H. Paniculata ‘Brussels Lace’ Interspecific Hybrids. J. Environ. Hortic. 2001, 19, 85–88. [Google Scholar] [CrossRef] [Scilit]
- Cai, M.; Wang, K.; Luo, L.; Pan, H.; Zhang, Q.; Yang, Y. Production of Interspecific Hybrids between Hydrangea Macrophylla and Hydrangea Arborescens via Ovary Culture. Hortscience 2015, 50, 1765–1769. [Google Scholar] [CrossRef] [Scilit]
- Nesi, B.; Ghiselli, L.; Gori, M.; Natale, R.; Tomiozzo, R.; Mansuino, A.; Biricolti, S. “In Vitro” Ovule Culture to Improve Genetic Variability in Hydrangea macrophylla. Horticulturae 2023, 9, 1028. [Google Scholar] [CrossRef] [Scilit]
- Feng, J.; Chen, S.; Chen, H.; Dai, L.; Qi, X.; Ahmad, M.Z.; Gao, K.; Qiu, S.; Jin, Y.; Deng, Y. Metabolomics Reveals a Key Role of Salicylic Acid in Embryo Abortion Underlying Interspecific Hybridization between Hydrangea macrophylla and H. arborescens. Plant Cell Rep. 2024, 43, 248. [Google Scholar] [CrossRef] [Scilit]
- Bak, S.; Han, T.-H. Evaluation of Genetic Diversity Using Simple Sequence Repeat Markers and Analysis of Cross Compatibility in Hydrangeas. Hortic. Environ. Biotechnol. 2024, 65, 1043–1052. [Google Scholar] [CrossRef] [Scilit]
- Schatlowski, N.; Köhler, C. Tearing down Barriers: Understanding the Molecular Mechanisms of Interploidy Hybridizations. J. Exp. Bot. 2012, 63, 6059–6067. [Google Scholar] [CrossRef] [Scilit]
- Alexander, L. Ploidy Level Influences Pollen Tube Growth and Seed Viability in Interploidy Crosses of Hydrangea macrophylla. Front. Plant Sci. 2020, 11, 100. [Google Scholar] [CrossRef] [Scilit]
- Beck, W.T.; Ranney, T.G. Ploidy Levels and Interploidy Hybridization in Panicle Hydrangea (Hydrangea paniculata). SNA Res. Conf. 2014, 59, 181–187. [Google Scholar]
- Tomato Genome Consortium. The Tomato Genome Sequence Provides Insights into Fleshy Fruit Evolution. Nature 2012, 485, 635–641. [Google Scholar] [CrossRef] [Scilit]
- Chen, S.; Lu, H.; Liu, H.; Si, M.; Cai, M.; Zhang, Q.; Yang, Y.; Zhang, D. Karyotype Analysis and Genome-Size Evaluation of Native Hydrangea Taxa in China. Hortscience 2025, 60, 1021–1025. [Google Scholar] [CrossRef] [Scilit]
- Nesi, B.; Lazzereschi, S.; Pecchioli, S.; Pacifici, S.; Venturieri, A.G.; Burchi, G. Development of Complementary Techniques Applied to Hydrangea Hybridizations. In Acta Horticulturae 1104: XXIX International Horticultural Congress on Horticulture: Sustaining Lives, Livelihoods and Landscapes (IHC2014): International Symposium on Ornamental Horticulture in the Global Greenhouse; International Society for Horticultural Science (ISHS): Leuven, Belgium, 2015; pp. 341–348. [Google Scholar] [CrossRef] [Scilit]
- Ketsa, S.; Wisutiamonkul, A.; Van Doorn, W.G. Auxin Is Required for Pollination-Induced Ovary Growth in Dendrobium Orchids. Funct. Plant Biol. 2006, 33, 887–892. [Google Scholar] [CrossRef] [Scilit]
- Rinehart, T.A.; Wadl, P.A.; Staton, M.E. An Update on Hydrangea macrophylla Breeding Targets and Genomics. In Acta Horticulturae 1191: III International Symposium on Woody Ornamentals of the Temperate Zone; International Society for Horticultural Science (ISHS): Leuven, Belgium, 2018; Volume 1191, pp. 217–224. [Google Scholar] [CrossRef] [Scilit]
- Raman, G.; Choi, K.-S.; Lee, E.M.; Morden, C.W.; Shim, H.; Kang, J.-S.; Yang, T.-J.; Park, S. Extensive Characterization of 28 Complete Chloroplast Genomes of Hydrangea Species: A Perspective View of Their Organization and Phylogenetic and Evolutionary Relationships. Comput. Struct. Biotechnol. J. 2023, 21, 5073–5091. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, X.; Zhang, X.; Xue, T.; Zhang, X.; Yang, F.; Yu, J.; Janssens, S.B.; Bussmann, R.W.; Yu, S. Phylogenomics and Historical Biogeography of Hydrangeeae (Hydrangeaceae) Elucidate the Effects of Geologic and Climatic Dynamics on Diversification. Proc. R. Soc. B Biol. Sci. 2023, 290, 20230659. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khaing, M.; Jung, H.; Kim, J.-B.; Han, T.-H. Characterization of Hydrangea Accessions Based on Morphological and Molecular Markers. Hortic. Sci. Technol. 2018, 36, 598–605. [Google Scholar] [CrossRef] [Scilit]
- Peng, J.Q.; Xu, Z.G.; Cao, F.X.; Dong, X.J.; Zhang, P.H. ISSR Analysis of Genetic Diversity in Cultivars of Hydrangea macrophylla and Hydrangea paniculata. Jiangsu Agric. Sci. 2017, 45, 5. [Google Scholar]
- Schenk, J.J.; Jacobs, S.; Hufford, L. Comparative Diversification Analyses of Hydrangeaceae and Loasaceae Reveal Complex Evolutionary History as Species Disperse out of Mesoamerica. Am. J. Bot. 2025, 112, e16455. [Google Scholar] [CrossRef] [Scilit]
- Granados Mendoza, C.; Wanke, S.; Goetghebeur, P.; Samain, M.-S. Facilitating Wide Hybridization in Hydrangea s. l. Cultivars: A Phylogenetic and Marker-Assisted Breeding Approach. Mol. Breed. 2013, 32, 233–239. [Google Scholar] [CrossRef] [Scilit]
- JaeBok, Y.; HyoGuen, P.; JaeBo, Y.; HyoGue, P. Trispecies Bridge Crosses, (Capsicum annuum x C. chinense) x C. baccatum, as an Alternative for Introgression of Anthracnose Resistance from C. baccatum into C. annuum. J. Korean Soc. Hortic. Sci. 2005, 46, 5–9. [Google Scholar]
- Mohanty, A.; Chrungu, B.; Verma, N.; Shivanna, K.R. Broadening the Genetic Base of Crop Brassicas by Production of New Intergeneric Hybrid. Czech J. Genet. Plant Breed. 2009, 45, 117–122. [Google Scholar] [CrossRef] [Scilit]
- Kubota, S.; Konno, I.; Kanno, A. Molecular Phylogeny of the Genus Asparagus (Asparagaceae) Explains Interspecific Crossability between the Garden Asparagus (A. officinalis) and Other Asparagus Species. Theor. Appl. Genet. 2012, 124, 345–354. [Google Scholar] [CrossRef] [Scilit]
- Birchler, J.A. Interploidy Hybridization Barrier of Endosperm as a Dosage Interaction. Front. Plant Sci. 2014, 5, 281. [Google Scholar] [CrossRef] [Scilit]
- Wang, W.H.; Wang, S.D.; Zhao, X.Y.; Li, X.Y.; Yu, J.J.; Chen, Z.H. Process of Pollen Sprouting and Pollen Tube Growth on the Lily Distant Hybridization. Acta Bot. Boreali–Occident. Sin. 2007, 27, 5. [Google Scholar]
- Bedinger, P.A.; Broz, A.K.; Tovar-Mendez, A.; McClure, B. Pollen-Pistil Interactions and Their Role in Mate Selection. Plant Physiol. 2017, 173, 79–90. [Google Scholar] [CrossRef] [Scilit]
- Broz, A.K.; Bedinger, P.A. Pollen-Pistil Interactions as Reproductive Barriers. Annu. Rev. Plant Biol. 2021, 72, 615–639. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.J. Callose in Plants. Bull. Biol. 2005, 40, 18–19. [Google Scholar]
- Wang, C.; Lei, J.J.; Jiang, C.; Xing, G.M. Study on Cross–Compatibility of Interspecific Hybridization and Selfing in Clivia Lindl. Sci. Agric. Sin. 2011, 44, 3822–3829. [Google Scholar]
- Xie, W.; Li, S.; Oba, E.; Peng, L.; Wang, J.; Zhang, L.; Song, J. Microscopic Observation and Transcriptome Analysis Provide Insights into Mechanisms of Hybrid Incompatibility in Rhododendron. Sci. Hortic. 2024, 336, 113417. [Google Scholar] [CrossRef] [Scilit]
- Raut, V.K.; Yadav, A.; Kaur, V.; Rao, M.; Pathania, P.; Wankhede, D.; Singh, M.; Singh, G.P. Pollen–Pistil Interactions in Divergent Wide Crosses Lead to Spatial and Temporal Pre-Fertilization Reproductive Barrier in Flax (Linum usitatissimum L.). Sci. Rep. 2025, 15, 6806. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mehmood, M.; Tanveer, N.A.; Joyia, F.A.; Ullah, I.; Mohamed, H.I. Effect of High Temperature on Pollen Grains and Yield in Economically Important Crops: A Review. Planta 2025, 261, 141. [Google Scholar] [CrossRef] [Scilit]
- Gawel, N.J.; Robacker, C.D. Effect of Pollen-Style Interaction on the Pollen Tube Growth of Gossypium hirsutum. Theor. Appl. Genet. 1986, 72, 84–87. [Google Scholar] [CrossRef] [Scilit]
- Gao, Q.; Wang, C.; Xi, Y.; Shao, Q.; Hou, C.; Li, L.; Luan, S. RALF Signaling Pathway Activates MLO Calcium Channels to Maintain Pollen Tube Integrity. Cell Res. 2023, 33, 71–79. [Google Scholar] [CrossRef] [Scilit]
- Lan, Z.; Song, Z.; Wang, Z.; Li, L.; Liu, Y.; Zhi, S.; Wang, R.; Wang, J.; Li, Q.; Bleckmann, A.; et al. Antagonistic RALF Peptides Control an Intergeneric Hybridization Barrier on Brassicaceae Stigmas. Cell 2023, 186, 4773–4787.e12. [Google Scholar] [CrossRef] [Scilit]
- Herrero, M.; Dickinson, H.G. Pollen Tube Growth Following Compatible and Incompatible Intraspecific Pollinations in Petunia hybrida. Planta 1980, 148, 217–221. [Google Scholar] [CrossRef] [Scilit]
- Sarla, N. Overcoming Interspecific Incompatibility in the cross Brassica campestris ssp. Japonica x Brassica oleracea Var. Botrytis Using Irradiated Mentor Pollen. Biol. Plant. 1988, 30, 384–386. [Google Scholar] [CrossRef] [Scilit]
- Fei, C.-H.; Tang, S.-S.; Shang, S.-H.; Dai, J.; Wang, X.-Y.; Wang, S.; Liu, W.-Q.; Wang, X.-F. Conspecific Pollen Advantage Mediated by the Extragynoecial Compitum and Its Potential to Resist Interspecific Reproductive Interference between Two Sagittaria Species. Front. Plant Sci. 2022, 13, 956193. [Google Scholar] [CrossRef] [Scilit]
- Carputo, D.; Frusciante, L.; Peloquin, S.J. The Role of 2n Gametes and Endosperm Balance Number in the Origin and Evolution of Polyploids in the Tuber-Bearing Solanums. Genetics 2003, 163, 287–294. [Google Scholar] [CrossRef] [Scilit]
- He, H.; Sadahisa, K.; Yokoi, S.; Tezuka, T. Parental Genome Imbalance Causes Hybrid Seed Lethality as Well as Ovary Abscission in Interspecific and Interploidy Crosses in Nicotiana. Front. Plant Sci. 2022, 13, 899206. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Yu, Y.; Chen, X.; Li, Y.; Jones, A.; Rose, R.J.; Ruan, Y.-L.; Song, Y. Mitigating Drought-Associated Reproductive Failure in Maize: From Physiological Mechanisms to Practical Solutions. Crop J. 2025, 13, 1022–1031. [Google Scholar] [CrossRef] [Scilit]
- Lentini, Z.; Restrepo, G.; Buitrago, M.E.; Tabares, E. Protocol for Rescuing Young Cassava Embryos. Front. Plant Sci. 2020, 11, 522. [Google Scholar] [CrossRef] [Scilit]
- N, P.; Parkash, C.; Bhatia, R.; Munshi, A.D.; Rao, M.; Subhasmita, S.; Behera, T.K.; Dey, S.S. An Efficient and Easy-to-Use Protocol for Induction of Haploids in Cucumber through Parthenogenic Embryo Development. Bot. Stud. 2024, 65, 30. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.