Article

Bioturbator Biodiversity Facets Show Differential Sensitivity to Sediment Trophic Status in Their Effects on Cross-Habitat Nutrient Cycling


by
Adriano Caliman
1,*,
André Luiz dos Santos Fonseca
2,
João José Fonseca Leal
3,
Rafael Dettogni Guariento
4,
Luciana Silva Carneiro
1 and
Francisco de Assis Esteves
5
1
Departamento de Ecologia, Universidade Federal do Rio Grande do Norte, Natal 59078-970, RN, Brazil
2
Instituto Federal Fluminense, Campus Cabo Frio 28909-971, RJ, Brazil
3
Instituto de Educação Ciência e Tecnologia do Rio de Janeiro (IFRJ), Campus Nilópolis 26530-060, RJ, Brazil
4
Centro de Ciências Biológicas e da Saúde, Universidade Federal de Mato Grosso do Sul, Campo Grande 79070-900, MS, Brazil
5
Instituto de Biodiversidade e Sustentabilidade, Universidade Federal do Rio de Janeiro, Macaé 27965-045, RJ, Brazil
*
Author to whom correspondence should be addressed.
Limnol. Rev. 2026, 26(3), 39; https://doi.org/10.3390/limnolrev26030039
Submission received: 6 June 2026 / Revised: 9 July 2026 / Accepted: 11 July 2026 / Published: 14 July 2026

Abstract

Biodiversity loss in aquatic ecosystems is accelerating, yet whether the effects of different biodiversity facets on biogeochemical processes are consistent or environmentally contingent remains poorly understood. Benthic invertebrate bioturbators drive nutrient exchange at the sediment–water interface of shallow aquatic ecosystems, but how sediment trophic status modulates the effects of their richness, identity, and composition on benthic–pelagic nutrient cycling is unclear. We conducted a factorial microcosm experiment using three functionally and phylogenetically distinct species—Campsurus melanocephalus (Ephemeroptera), Heteromastus similis (Polychaeta), and Heleobia australis (Gastropoda)—assembled as monocultures, bicultures, and tricultures across a gradient of sediment organic matter concentration ([OM]) representative of natural variability in a neotropical coastal lagoon. Species richness produced a consistent, saturating enhancement of NH3 fluxes that was independent of sediment trophic status, while species identity strongly differentiated monoculture effects in a pattern that was likewise stable across the [OM] gradient. In contrast, although biculture compositions did not differ from one another across the [OM] gradient, the overall magnitude of biculture-mediated NH3 fluxes increased with sediment trophic status, suggesting that multispecies assemblage effects are more responsive to environmental context than those of single species. These findings reveal that biodiversity facets diverge not only in how strongly they affect ecosystem functioning, but also in how sensitive their effects are to environmental variation. We therefore conclude that predicting benthic–pelagic nutrient exchange in shallow coastal ecosystems requires considering both the biological structure of bioturbator assemblages and the organic matter context of the sediment.

1. Introduction

Biodiversity’s role in ecosystem functioning represents one of ecology’s fundamental inquiries [1]. Despite initial controversy, meta-analytical and quantitative syntheses have established that biodiversity substantively influences the magnitude and the stability of individual and multiple ecosystem processes [2,3,4,5,6]. Two primary mechanistic explanations have emerged for these biodiversity–ecosystem function relationships: the sampling effect, wherein species-rich communities are statistically more likely to contain functionally dominant taxa [7,8,9], and complementarity effects, wherein niche partitioning and facilitation enable diverse communities to utilize environmental resources more efficiently [10,11].
Research efforts examining biodiversity–ecosystem function relationships have been asymmetrically distributed across ecosystems, community types and ecosystem processes, with terrestrial plant communities and primary productivity receiving disproportionate attention [12]. Additionally, the cross-habitat effects of biodiversity loss have been considerably underexplored, constraining our understanding of how biodiversity loss or alteration within a given habitat or ecosystem may scale up to adjacent habitats or ecosystems [13]. Concomitantly, biodiversity loss proceeds at an accelerated rate in aquatic ecosystems, particularly affecting higher trophic levels and consumer communities [14,15,16,17]. This discrepancy underscores the imperative to expand biodiversity–ecosystem function research beyond terrestrial primary producers to encompass aquatic ecosystems [18,19]. Such expansion is particularly important for regenerative ecosystem processes, including nutrient cycling, which are strongly mediated by consumer communities in aquatic ecosystems [20,21].
Lentic ecosystems present ideal systems for investigating biodiversity effects on cross-habitat ecosystem processes [22], particularly through the mechanism of bioturbation—the modification of sediment physical properties through organism movement and foraging activities [23,24,25]. Bioturbation mediates regenerative processes, facilitates nutrient translocation between ecosystem compartments and constitutes a crucial component of aquatic nutrient cycling [26,27] and carbon fluxes within and between aquatic environments and the atmosphere [28,29,30]. Benthic invertebrates, with their immense taxonomic, functional and phylogenetic diversities, represent quintessential ecosystem engineers that drive this bioturbation process [31,32,33,34]. Their relatively low functional redundancy [27,35] allows researchers to distinguish between taxonomic and functional diversity effects, providing crucial insights into biodiversity’s multifaceted importance for ecosystem functioning [36,37].
Empirical evidence demonstrates that benthic invertebrate diversity significantly influences nutrient flux across the sediment–water interface [38,39,40,41,42]. However, these biodiversity effects can be strongly context-dependent, varying among diverse ecological settings [43,44]. Particularly understudied is how environmental characteristics, specifically resource availability or trophic status, interact with bioturbator diversity to affect nutrient cycling [45]. Research across various ecological communities indicates that resource availability can either amplify or nullify biodiversity effects on ecosystem processes [46,47,48,49]. Yet, limited information exists regarding how sediment trophic status, an important component of habitat structure and heterogeneity of the sedimentary environment, might modulate the magnitude and directionality of benthic bioturbator diversity effects on nutrient recycling [50].
This knowledge deficiency is particularly relevant given that benthic sedimentary habitats exhibit substantial heterogeneity in trophic status both across systems [51] and within individual ecosystems [52]. Littoral sediments typically contain higher organic content than profundal limnetic regions due to macrophyte and riparian inputs [53,54], while point-source pollution can create pronounced spatial heterogeneity in sediment trophic status [55,56]. Previous studies have demonstrated that individual bioturbator species’ effects on nutrient cycling vary in response to sediment organic content [45,50], suggesting that sediment trophic status may similarly influence interspecific interactions among bioturbators. This expectation is mechanistically plausible because sediment organic matter represents both a basal resource for deposit-feeding invertebrates and a major driver of microbial activity, oxygen demand, and redox conditions within sediments. Changes in sediment [OM] may therefore alter the behavior, vertical distribution, feeding activity, and bioirrigation intensity of bioturbator species [57,58,59]. Consequently, sediment trophic status may modify not only the effects of individual species, but also the strength and direction of species interactions that emerge in multispecies assemblages, ultimately influencing nutrient fluxes across the sediment–water interface [50]. However, whether sediment trophic status modulates the effects of multiple bioturbator biodiversity facets (i.e., species richness, species identity, and species composition) on nutrient fluxes remains poorly understood. Addressing this gap would improve our understanding of the spatial variability of biodiversity effects and strengthen the extrapolation of laboratory findings to broader ecological scales [60,61,62].
Here, we conducted a laboratory microcosm experiment to examine whether and how sediment trophic status modifies the effects of bioturbator biodiversity on nutrient flux (ammonia—NH3) across the sediment–water interface. Specifically, we addressed three questions. First, does bioturbator species richness (i.e., effects of species number on ecosystem functioning) affect NH3 flux, and does this effect vary across sediment trophic status levels? Second, does species identity (i.e., species-specific effects on ecosystem functioning) affect NH3 flux, and are these effects dependent on sediment trophic status? Third, does species composition (i.e., effects of species interactions on ecosystem functioning) affect NH3 flux, and does sediment trophic status alter these effects? NH3 was selected as the response variable because it is a sensitive indicator of microbial mineralization of organic nitrogen and represents a key nutrient for primary production in coastal lagoons. In addition, NH3 flux across the sediment–water interface is strongly influenced by benthic bioturbators [33,38,43], whose reworking and bioirrigation activities can enhance organic matter decomposition and promote nutrient transfer from sediments to the overlying water [57,58,59]. We hypothesized that sediment [OM] would modulate the effects of invertebrate bioturbator species richness, species identity, and species composition on benthic–pelagic nutrient exchange.

2. Materials and Methods

2.1. Study Site Characterization

The sediment, water, and benthic macroinvertebrate organisms utilized in this experiment were sampled in Imboassica lagoon, a freshwater coastal lagoon situated within the urban area of Macaé municipality on the northern coast of Rio de Janeiro State (22°24′35″ S and 41°49′10″ W) in Brazil. The Imboassica lagoon exists within the geomorphological domain of an alluvial sedimentation plain, with genesis dating to the Tertiary period [63]. This ecosystem exemplifies a quintessential neotropical coastal lagoon segregated from the marine environment by a sand barrier [64]. The lagoon encompasses approximately 3.26 km2, with a mean depth of 1.09 m [65]; has been characterized as a eutrophic and highly productive coastal lagoon [66]; and contains sediment characterized by substantial organic matter concentrations [67]. Both its inorganic constituents (clays, silts, and fine sand) and organic composition demonstrate pronounced spatial heterogeneity [68]. Given its location within the urban perimeter, the Imboassica lagoon is subjected to multiple anthropogenic perturbations, including untreated domestic effluent discharge [69]. These anthropogenic activities have been promoting increasing burial rates of carbon, nitrogen and phosphorus in the sediment of Imboassica lagoon during the past several decades [67].

2.2. Benthic Invertebrate Species Studied

For this study, we used 3 functionally different benthic invertebrate species that are the most abundant at the studied site and have distinct modes of bioturbatory activities within the sediment. The species pool we used was therefore ecologically representative of the local benthic community while also encompassing functionally contrasting bioturbation strategies, allowing us to test whether sediment trophic status modulates biodiversity effects across a biologically meaningful range of bioturbator functional traits. Nymphs of Campsurus melanocephalus (Ephemeroptera, Polymitarcidae) can be functionally categorized as tube filter feeders [70]. C. melanocephalus constructs tubes within the sediment that exhibit morphological variability, predominantly assuming U or J configurations, with variable depth penetration. The organism generates water flow through these tubes via corporeal undulations, thereby satisfying respiratory requirements while simultaneously filtering particulate organic matter and microorganisms. C. melanocephalus nymphs attain lengths of up to 3 cm and facilitate water circulation through their tubes via metachronal undulations of abdominal gills [70]. This behavioral adaptation enhances oxygen diffusion into deep, anoxic sediment strata while facilitating nutrient exchange across the sediment–water interface [71,72].
The species Heteromastus similis (Polychaeta, Capitellidae) is distinguished by its construction of semi-permanent, irregular tubes within the sediment and its consumption of detrital material transported from oxic surface layers to deeper sediment horizons. Representatives of the family Capitellidae are functionally classified as sub-surface deposit feeders [28]. Mature H. similis specimens measure approximately 1 mm in diameter and may reach lengths of 15 cm [73], though specimens collected from the Imboassica lagoon typically range from 3 to 5 cm. Capitellidae family members possess physiological adaptations enabling tolerance to elevated sulfide concentrations and hypoxic conditions [74], facilitating exploration of deep sediment strata without necessitating active water circulation [75]. Their feeding strategy involves consumption of organic particles, either isolated or adhered to sediment particulates. They deposit fecal material in the form of pelleted aggregates along their tubes or on the sediment surface, rendering them significant translocators of organic and inorganic constituents between discrete sediment strata without inducing substantial alterations to sediment oxidation–reduction dynamics [76,77].
H. australis (Gastropoda, Hydrobiidae) inhabits the sediment surface, primarily consuming recently deposited detrital material, and is frequently observed in association with aquatic macrophytes, feeding on periphyton [78]. This ecological niche, characteristic of other Hydrobiidae family representatives, is constrained to the sediment surface primarily due to sensitivity to oxygen-depleted conditions, thus functionally categorized as a surface deposit feeder [75]. Adult H. australis specimens reach maximum lengths of 5 mm and constitute the predominant benthic invertebrate species in the Imboassica lagoon [67,68].

2.3. Field and Laboratory Procedures

Sediment and benthic invertebrates were collected using core samplers according to protocols established by Ambühl and Bührer (1975) [79], focusing on the central region of Imboassica Lagoon. This sampling location was selected because its high sediment [OM] provided the necessary starting condition to generate the experimental trophic gradient in the sediment (see below). This location also harbors well-developed benthic populations and higher benthic invertebrate species diversity [67,80]. The experiment used only the upper 10 cm of sediment, which corresponds to the stratum where benthic organisms are most concentrated and where microbial activity is expected to be most intense [81].
A portion of the collected sediment was carefully sorted in the field using sieves, and the target benthic invertebrate species were transferred to species-specific polystyrene thermal containers containing native sediment and lagoon water. In the laboratory, organisms were maintained under constant aeration for acclimatization until the beginning of the experiment. A second portion of the remaining sediment was sieved in the laboratory through a 1 mm mesh to remove macrofauna, shell fragments, and particulate material that, according to Reise (2002) [75], may inhibit macroinvertebrate movement and distribution within the sediment. The sieved sediment was then homogenized and subjected to freeze–thaw cycling to eliminate remaining infauna, including small individuals and resistant resting stages as eggs or cysts. This procedure generated the defaunated natural sediment used as the base sediment in the experimental treatments, while allowing the comprehensive elimination of metazoans [38]. We acknowledge that freeze–thaw cycling may also reduce most of the sediment microbial community. However, potential effects on microbial activity were minimized by the subsequent sediment stabilization period, during which microbial activity and biogeochemical gradients were allowed to partially re-establish before the incubations, as detailed in Section 2.4.
A third portion of the remaining sediment was used to produce the organic matter-free mineral fraction later used to manipulate sediment [OM]. To obtain this mineral fraction, sediment was incinerated at 550 °C for 4 h to eliminate organic matter and subsequently washed with distilled water to remove residual ash and soluble compounds. This procedure yielded an organic matter-free mineral fraction while retaining the original sediment granulometry as much as possible. The experimental sediments were therefore prepared by mixing, when applicable, this organic matter-free mineral fraction with the previously sieved, homogenized, and freeze–thawed natural sediment (see below).

2.4. Experimental Design and Setup

The experiment was designed to test how sediment [OM] modifies the effects of benthic invertebrate species richness, identity, and composition on NH3 fluxes in microcosms containing a sediment–water interface. For this, the three target species, H. similis, C. melanocephalus, and H. australis, were assembled as monocultures, bicultures, and tricultures across three experimental levels of sediment [OM]. The design also included controls without animals for each sediment [OM] level, consisting of microcosms with only sediment and lagoon water, to estimate diffusional NH3 fluxes. Monocultures consisted of the three single-species treatments, and bicultures consisted of all three possible pairwise species combinations. Each monoculture and biculture treatment was established with three replicates per sediment [OM] level, whereas the triculture treatment, consisting of the single three-species combination, was established with nine replicates per sediment [OM] level. Controls were also established with three replicates per sediment [OM] level. In total, the experiment consisted of 90 microcosms. This balanced design ensured equivalent replication of the main biological factors within each sediment [OM] level. Species richness was represented by the same number of fauna-containing microcosms across monoculture, biculture, and triculture treatments, while species identity within monocultures and species composition within bicultures were represented by all possible treatments with equal replication. Thus, species richness, identity, and composition effects, as well as their interaction with sediment [OM], could be evaluated under a fully balanced experimental structure [82,83,84,85].
The sediment [OM] factor was manipulated by diluting the previously sieved, homogenized, and freeze–thawed natural sediment described above with the organic matter-free mineral sediment fraction. To determine the appropriate proportions of mineral sediment addition relative to natural sediment dry weight, sediment water content was estimated from wet–dry weight differences. A wet-to-dry conversion factor was then applied to calculate the required amount of mineral fraction to be added, enabling controlled dilution of sediment [OM] to the target levels. Three sediment [OM] conditions were established: unaltered prepared natural sediment, representing the highest sediment [OM] condition (High); prepared natural sediment mixed with 50% mineral sediment on a dry weight basis, representing the intermediate sediment [OM] condition (Medium); and prepared natural sediment mixed with 75% mineral sediment on a dry weight basis, representing the lowest sediment [OM] condition (Low). This methodology generated an effective sediment [OM] gradient within the spatial [OM] variability observed in Imboassica Lagoon [67,86]. Importantly, establishing this gradient experimentally by diluting a common natural sediment avoided potential confounding effects that would arise from collecting sediments with contrasting [OM] from different areas of the lagoon. In such a field-based approach, variation in sediment [OM] would likely be accompanied by uncontrolled differences in other sediment properties, such as grain-size structure, microbial community composition, and other local physicochemical conditions. Because the mineral fraction used for dilution was obtained from the same sediment and processed to retain its original granulometry as much as possible, our approach allowed sediment [OM] to be manipulated while minimizing changes in grain-size structure. This is an important methodological advantage, given that sediment granulometry can influence the effects of invertebrate bioturbation. In addition, establishing the [OM] gradient through sediment dilution, rather than through organic matter addition, avoids some limitations of enrichment-based methods. Organic matter addition often involves material in different degradation states, and therefore with qualitative differences from endogenous sediment organic matter, potentially generating hostile physicochemical conditions for invertebrate fauna [45]. This effect would be particularly pronounced in Imboassica Lagoon, which is characterized by elevated mean sediment [OM] [67].
After the sediment [OM] treatments were prepared, they were stabilized before the start of the experiment. Ten days before incubation, each prepared sediment [OM] treatment was placed in separate aquaria (40 × 40 × 30 cm), forming a sediment layer of approximately 10 cm. The sediments were then covered with previously filtered Imboassica Lagoon water (GF/C 1.2 µm, Whatman, Maidstone, UK) to stabilize and re-establish the microbial community and biogeochemical gradients [38,87]. The aquaria were kept aerated and in the dark until the start of the experiment. Hours before incubation began, acrylic core microcosms (20 cm height × 4 cm diameter) were inserted into the stabilized sediments, establishing a 10 cm sediment and a 9 cm overlying water column in each microcosm with minimal disturbance of the vertical structure. The overlying water column was then drained and gently replaced with filtered Imboassica Lagoon water (GF/F 0.7 µm, Whatman), to reduce the remaining nutrients from the stabilization period.
The biological treatments were then assembled according to the experimental design. The total biomass of benthic macroinvertebrates in each fauna-containing microcosm was standardized at 300 mg wet weight, which is near the average benthic community biomass observed per unit area at the study site [80]. Biomass partitioning among species followed a substitutive design, adhering to a factorial replacement series protocol [82,83], in which species-specific biomass within treatments was proportionally divided by the number of constituent species. Live individuals of each species were weighed to 0.1 mg precision after removing excess water with absorbent paper and were immediately distributed into the microcosms. Throughout the experiment, microcosms were maintained under continuous aeration, in the dark, and at a constant temperature (25–27 °C), minimizing O2 and nutrient stratification and preventing photosynthetic nutrient uptake. Water samples of 20 mL were collected at the beginning of the experiment and after 48 h of incubation, filtered (GF/F 0.7 µm, Whatman), and frozen for later determination of NH3 concentrations.

2.5. Analytical Chemistry Protocols and Nutrient Flux Calculation

Dissolved ammonia/ammonium concentrations in the water samples were determined using the indophenol blue colorimetric method as described by Koroleff (1978) [88]. The concentrations of OM, total carbon (TC), total nitrogen (TN) and total phosphorus (TP) were determined for each experimental level of sediment trophic state. Sediment [OM] was estimated gravimetrically by loss on ignition, based on the difference between sediment dry weight and sediment weight after calcination at 550 °C for 4 h [89]. TC and TN sediment concentrations were determined from dried and homogenized sediment samples using a Carlo Erba elemental analyzer, based on high-temperature combustion of the sample and subsequent quantification of the combustion products. TP sediment concentration was determined after acid digestion of dried sediment samples, followed by colorimetric blue-method quantification of phosphorus in the digest. All sediment OM, TC, TN, and TP concentrations were determined in triplicate and expressed as % of sediment dry weight.
NH3 fluxes across the sediment–water interface were calculated from the change in dissolved NH3 concentration during the 48 h incubation. For each microcosm, the difference between final and initial NH3 concentration was multiplied by the overlying water volume and then divided by the sediment surface area of the microcosm and by the incubation time, yielding fluxes expressed as µmol m−2 h−1 according to the formula:
NH3 flux = [(NH3-final − NH3-initial) × V]/(A × t)
where NH3-final and NH3-initial are the final and initial NH3 concentrations in the overlying water, respectively, expressed as µmol L−1; V is the overlying water volume in liters; A   is the sediment surface area of the microcosm in m2; and t   is the incubation time in hours. To estimate NH3 fluxes mediated by faunal bioturbation, the flux calculated for each fauna-containing microcosm was corrected by subtracting the mean flux obtained from the corresponding control microcosms established at the same sediment [OM] level. Because NH3 fluxes were corrected by subtracting the mean flux of sediment-only controls within each sediment [OM] level, corrected fluxes represent the net contribution of faunal bioturbation to NH3 release beyond the background flux generated by the sediment itself. Therefore, any subsequent effect of sediment [OM] detected on corrected NH3 fluxes reflects variation in the bioturbation-mediated component of NH3 release across the sediment trophic gradient, rather than differences in basal sediment NH3 diffusion alone. Thus, positive corrected fluxes indicate increased NH3 release associated with benthic fauna relative to sediment-only controls, whereas negative values indicate lower NH3 release or greater NH3 retention relative to controls.

2.6. Statistical Analysis

To evaluate the individual and interactive effects of the benthic invertebrate biodiversity facets and sediment [OM] levels on NH3 fluxes, we used a set of complementary analysis of variance models. This approach was adopted because species richness, species identity, and species composition represent different biodiversity facets that are most appropriately evaluated at different levels of experimental design. Species richness effects were assessed across the three richness levels, whereas species identity effects were evaluated among monocultures and species composition effects among bicultures.
Prior to analysis, NH3 flux data were log10-transformed to improve compliance with the assumptions of analysis of variance. Model assumptions were evaluated on the transformed data. Normality was assessed by visual inspection of Q–Q plots and by Shapiro–Wilk tests applied to model residuals, whereas homogeneity of variances was assessed by residual-versus-fitted plots and Levene’s tests. No severe departures from ANOVA assumptions were detected after transformation. The effects of sediment [OM] and species richness were first tested using a two-way factorial ANOVA including sediment [OM], species richness, and their interaction as fixed categorical factors. In this model, sediment [OM] had three levels (Low, Medium, and High), and species richness had three levels, corresponding to one, two, and three species, represented by monocultures, bicultures, and tricultures, respectively. Because the experimental design provided the same number of fauna-containing microcosms for each richness level within each sediment [OM] level, this model allowed richness effects and richness × sediment [OM] interactions to be tested under a balanced structure.
Species identity effects were tested in a separate ANOVA restricted to monoculture treatments. In this model, sediment [OM], species identity, and the sediment [OM] × species identity interaction were included as fixed factors. This analysis tested whether NH3 flux differed among the three single-species treatments and whether species-specific effects varied across the sediment [OM] gradient. Species composition effects were evaluated in an analogous ANOVA restricted to biculture treatments, with sediment [OM], species composition, and the sediment [OM] × species composition interaction included as fixed factors. This model tested whether NH3 flux differed among the three pairwise species combinations and whether these compositional effects depended on sediment [OM].
Whenever significant effects were detected by ANOVA, Tukey’s HSD post hoc tests were used to identify differences among factor levels. All analyses were performed in Statistica version 10.0 for Windows, using a significance level of α = 0.05.

3. Results

The sediment dilution procedure produced the expected gradient in sediment trophic status. Organic matter content was highest in the unaltered natural sediment, intermediate in the 50% mineral sediment dilution treatment, and lowest in the 75% mineral sediment dilution treatment. The same decreasing pattern was observed for TC, TN, and TP contents, confirming that the experimental manipulation generated sediments with progressively lower organic and nutrient contents from the High to the Low trophic status levels (Table 1).
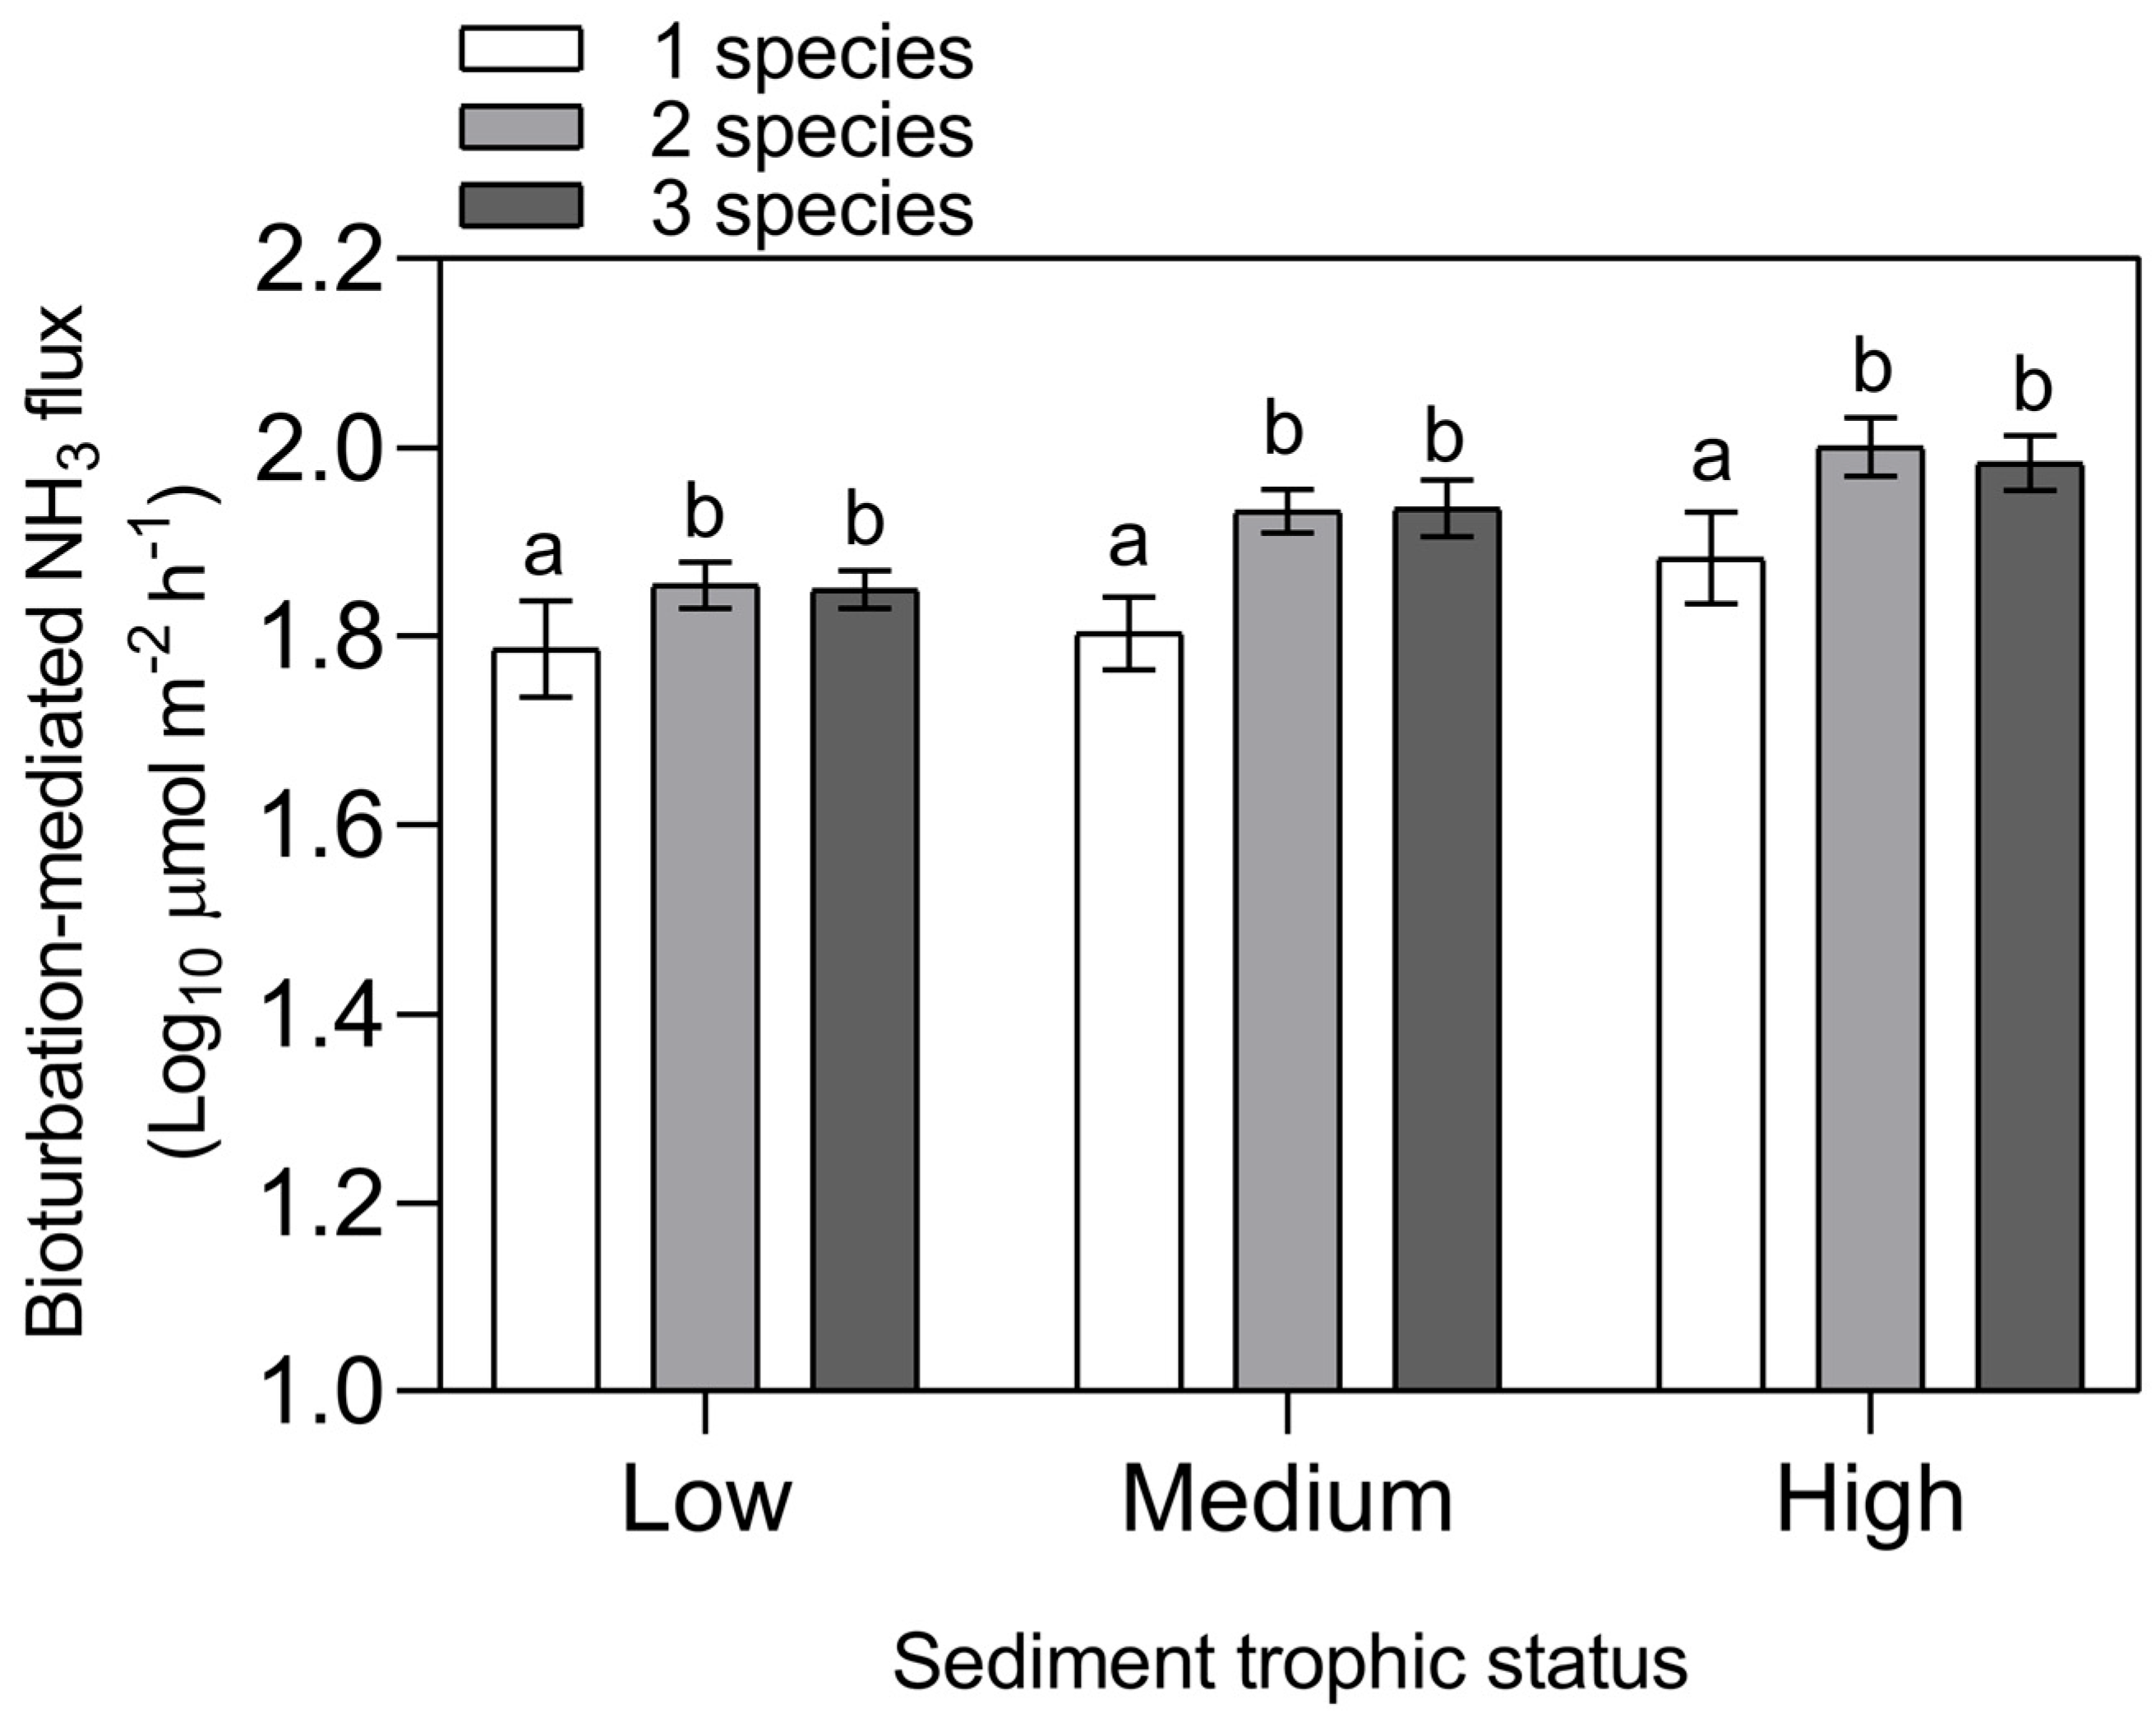
Bioturbation-mediated NH3 fluxes varied with both sediment trophic status and bioturbator species richness, but no interactive effect between these factors was detected (Table 2; Figure 1). The factorial ANOVA showed significant individual effects of sediment trophic status and species richness, whereas the sediment trophic status × species richness interaction was not significant (Table 2). Overall, bioturbation-mediated NH3 fluxes increased along the sediment trophic status gradient, with higher values in the High sediment [OM] treatment than in the Low treatment. Across all sediment trophic status levels, monocultures showed lower NH3 fluxes than bicultures and tricultures, while bicultures and tricultures did not differ from each other according to Tukey post hoc comparisons. This pattern indicates a consistent saturating effect of bioturbator species richness on NH3 flux, with an increase from one to two species but no further increase from two to three species, regardless of sediment trophic status.
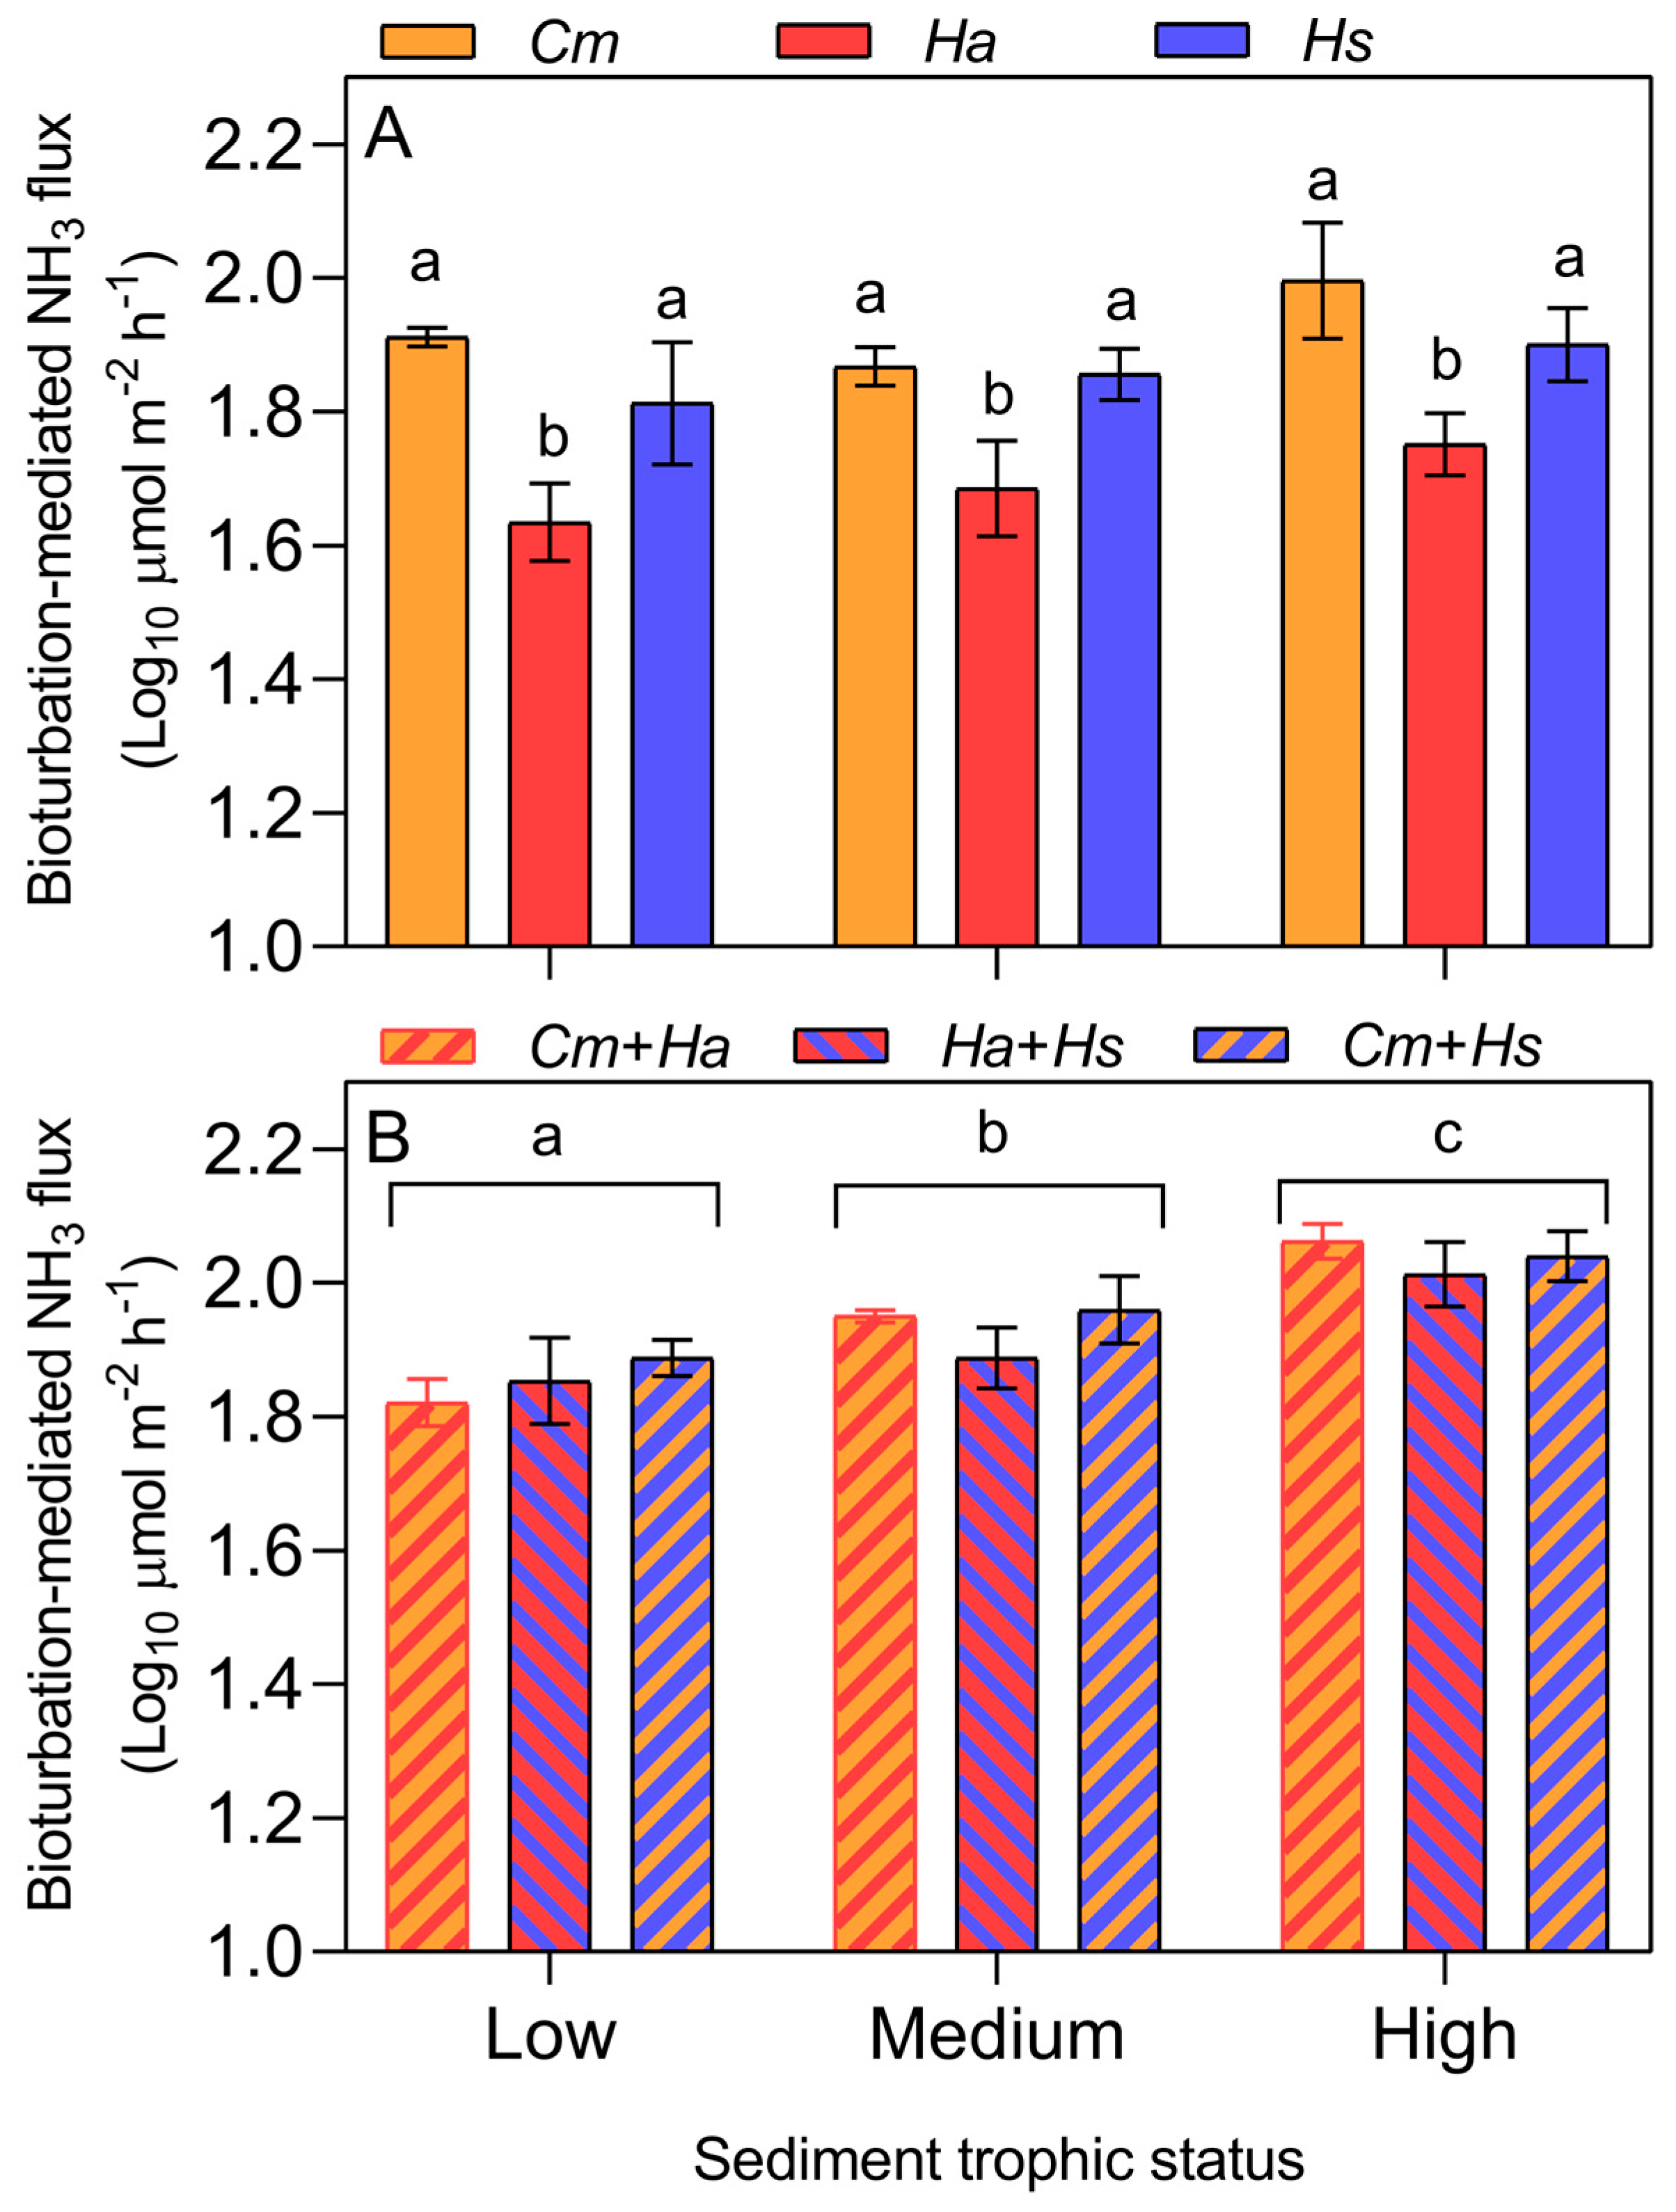
Bioturbation-mediated NH3 fluxes differed among species identities when analyses were restricted to monocultures, but did not vary significantly among sediment trophic status levels, and no trophic status × species identity interaction was detected (Table 3a; Figure 2A). Species identity had a significant effect on NH3 flux, whereas sediment trophic status and the trophic status × species identity interaction were not significant (Table 3a), indicating that differences among monocultures were consistent across the sediment [OM] gradient. Across all sediment trophic status levels, H. australis monocultures showed lower NH3 fluxes than C. melanocephalus and H. similis monocultures, while the latter two species did not differ from each other according to Tukey post hoc comparisons.
In contrast, when analyses were restricted to bicultures, sediment trophic status significantly affected bioturbation-mediated NH3 fluxes, whereas species composition showed a marginal but non-significant effect, and the trophic status × species composition interaction was not significant (Table 3b; Figure 2B). Thus, unlike the pattern observed for monocultures, biculture-mediated NH3 fluxes varied along the sediment trophic status gradient, with higher fluxes under High sediment trophic status. However, the three biculture compositions showed similar NH3 fluxes within each sediment trophic status level.

4. Discussion

Our results show that sediment trophic status and bioturbator biodiversity both influence NH3 fluxes across the sediment–water interface, but that different facets of biodiversity differed in their individual effects and in their apparent sensitivity to sediment [OM]. Species richness produced a consistent, saturating increase in bioturbation-mediated NH3 fluxes, with higher fluxes in bicultures and tricultures than in monocultures, but with no further increase from bicultures to tricultures. Species identity also affected NH3 fluxes among monocultures, indicating that the three bioturbator species were not functionally equivalent in their individual effects on benthic–pelagic nutrient exchange. However, neither the richness effect nor the identity effect varied significantly across sediment trophic status levels. In bicultures, sediment trophic status increased NH3 fluxes, whereas species composition showed only a marginal effect and did not interact significantly with sediment [OM]. Therefore, our initial hypothesis that sediment [OM] would modulate the effects of multiple facets of bioturbator biodiversity was only partially supported. More broadly, these findings suggest that biodiversity facets may differ not only in how strongly they affect ecosystem functioning, but also in how their effects are expressed across environmental contexts.
Understanding whether biodiversity effects are consistent or context-dependent is central to biodiversity–ecosystem functioning research, because environmental variation can alter the mechanisms through which species affect ecosystem processes [43,44,90,91]. Resource availability is especially relevant in this regard because it can modify the balance between dominance, complementarity, facilitation, and competition among species [7,8,9,10,11,46,47,48,49,92]. Evidence from aquatic and benthic systems shows that disturbance regimes, flow conditions, habitat structure, and abiotic context can alter the magnitude and detectability of biodiversity effects on ecosystem functioning [50,93,94,95,96]. Spatial heterogeneity can further modify biodiversity–function relationships by changing the range of microhabitats, resource patches, and functional opportunities available to organisms [97]. In sedimentary aquatic habitats, this issue is particularly important because sediment organic matter is spatially heterogeneous both among ecosystems and within individual water bodies [51,52,53,54,55,56]. Such variation may influence microbial activity, oxygen demand, redox gradients, resource availability for deposit feeders, and behavioral responses of benthic fauna [32,45,57,58,59]. Our experiment contributes to this broader discussion by showing that sediment [OM] can affect the magnitude of NH3 fluxes mediated by bioturbation, while some biodiversity effects, especially richness and identity effects, remain relatively consistent across a realistic gradient of sediment trophic status.
The positive effect of species richness on NH3 fluxes is consistent with previous evidence that benthic invertebrate diversity can enhance nutrient exchange and other ecosystem processes at the sediment–water interface [38,39,40,98,99,100,101]. However, the shape of this response was clearly saturating: increasing richness from one to two species increased NH3 fluxes, but adding a third species did not produce a further increase. This pattern suggests that the main functional increase occurred when assemblages shifted from single-species effects to multispecies assemblages, whereas two-species assemblages were already sufficient to generate fluxes comparable to those observed in tricultures. Such a saturating response is compatible with partial functional complementarity among species, but also with some degree of functional redundancy once key bioturbation modes are represented in the assemblage. The species used in this experiment differ markedly in their functional roles, including tube construction and bioirrigation by C. melanocephalus, subsurface deposit feeding and sediment translocation by H. similis, and surface deposit feeding by H. australis [70,71,72,73,74,75,76,77,78]. These differences likely increased the range of sediment layers, particles, and microhabitats influenced by multispecies assemblages. Nevertheless, the absence of a further increase from bicultures to tricultures indicates that the relationship between richness and nutrient flux was not linear and that the measured process may become functionally saturated at relatively low levels of bioturbator richness.
The absence of a sediment [OM] × species richness interaction is also important. Because sediment [OM] affects both the quantity of organic resources and the physicochemical conditions under which benthic organisms operate, we expected richness effects to vary across the sediment trophic gradient. Instead, the richness effect was consistent across Low, Medium, and High sediment [OM] conditions. This result suggests that, within the range of sediment [OM] tested here, the mechanisms by which multispecies assemblages generated higher NH3 fluxes than monocultures were robust to variation in sediment trophic status. In other words, sediment [OM] increased the overall magnitude of bioturbation-mediated NH3 fluxes but did not change the relative difference among richness levels. This distinction is important because the fluxes analyzed here were corrected by the corresponding sediment-only controls. Therefore, the positive effect of sediment trophic status on corrected fluxes cannot be attributed simply to greater basal NH3 diffusion from more organic-rich sediments. Rather, it indicates that the net contribution of faunal activity to NH3 release increased under higher sediment [OM]. Thus, sediment trophic status modulated the average effect of bioturbation itself, even though this modulation was not expressed as a significant richness × sediment [OM] interaction.
Species identity strongly affected NH3 fluxes in monocultures, indicating that the three bioturbator species were not functionally interchangeable in their effects on benthic–pelagic nutrient exchange. Although we did not directly quantify the specific behavioral mechanisms underlying these differences, the result is consistent with the broader view that bioturbator effects on benthic–pelagic nutrient flux depend on species-specific traits related to sediment use, feeding activity, particle reworking, and bioirrigation [26,27,31,32,33,34,100,102]. Thus, our findings reinforce that species identity is an important biodiversity facet for predicting how benthic macroinvertebrates influence nutrient fluxes across the sediment–water interface. In our experiment, H. australis monocultures produced lower NH3 fluxes than monocultures of C. melanocephalus and H. similis. This pattern is consistent with their contrasting modes of sediment use. H. australis is mainly associated with the sediment surface and is functionally categorized as a surface deposit feeder, whereas C. melanocephalus constructs tubes and actively ventilates them, and H. similis explores deeper sediment layers as a subsurface deposit feeder [70,71,72,73,74,75,76,77,78]. Species that move, feed, or irrigate deeper sediment layers are expected to have stronger effects on solute transport, redox coupling, and microbial processes across the sediment–water interface than species whose activity is mostly restricted to the sediment surface [32,34,57,58,59,100,102].
Although species identity affected NH3 fluxes, these identity effects did not vary significantly across the sediment [OM] gradient. This indicates that differences among monocultures were relatively stable across sediment trophic status levels. This result contrasts with the expectation that increasing sediment [OM] would amplify differences among species by altering resource availability, oxygen demand, or the need for bioirrigation. One possible interpretation is that species-specific bioturbation modes imposed relatively consistent constraints on NH3 fluxes across the tested [OM] range. For instance, surface activity by H. australis may remain less effective at enhancing sediment–water nutrient exchange regardless of sediment [OM], whereas tube-building or deeper sediment exploration by C. melanocephalus and H. similis may maintain higher fluxes across the same gradient. Thus, in monocultures, functional identity appeared to dominate over environmental modulation by sediment trophic status.
The pattern observed in multispecies treatments adds an important nuance. In bicultures, sediment trophic status significantly affected NH3 fluxes, with higher fluxes under the High sediment [OM] condition, whereas species composition showed only a marginal effect and did not interact significantly with sediment [OM]. Together with the richness analysis, in which bicultures and tricultures consistently showed higher fluxes than monocultures across the sediment [OM] gradient, this pattern suggests that multispecies assemblages maintained a functional advantage over monocultures under all sediment trophic conditions, while the absolute magnitude of their bioturbation-mediated NH3 release increased in more organic-rich sediments. Because corrected fluxes subtract the corresponding sediment-only controls, this increase reflects a stronger net faunal contribution to NH3 release, not simply greater nutrient availability in the sediment. Thus, the individual effects of species were relatively insensitive to sediment [OM], whereas the realized effects of multispecies assemblages appeared more responsive to sediment trophic status. This does not provide formal evidence of complementarity or non-additive interactions, which would require comparing observed mixture effects with expected effects derived from monocultures within each sediment [OM] level. However, it is consistent with the idea that interactions among species, or the combined expression of different bioturbation modes, can make assemblage-level effects more responsive to environmental context than single-species effects [45,103,104,105,106,107].
Several mechanisms may explain why sediment trophic status affected biculture fluxes but not monoculture fluxes. Multispecies assemblages can increase the spatial and functional extent of sediment reworking by combining different modes of sediment use, feeding, burrowing, and bioirrigation [26,27,32,34,98,99,100,101,102]. Under higher sediment [OM], this broader functional activity may interact with increased organic substrate availability, microbial biomass, or stronger redox gradients, resulting in greater NH3 release to the water column. In contrast, monocultures may be constrained by the particular behavior and sediment-use pattern of a single species. Species interactions may also alter the functional expression of traits, because the realized effects of a species on sediment properties can depend on the presence, density, or dominance of other species [45,105,106,107]. However, because we did not directly measure organism movement, burrow structure, oxygen profiles, microbial activity, or mineralization rates, these mechanisms should be interpreted as plausible explanations rather than direct evidence. Future studies combining biodiversity manipulations with direct measurements of bioturbation intensity, bioirrigation, oxygen penetration, and microbial processes would help clarify how species interactions and sediment trophic status jointly affect nutrient regeneration.
An important methodological aspect of our study is that sediment [OM] was manipulated by diluting a common natural sediment with an organic matter-free mineral fraction obtained from the same sediment, rather than by collecting sediments from different areas of the lagoon or by adding external organic matter. This design reduces confounding effects that would arise if natural sediments with different [OM] also differed in granulometry, microbial community composition, contaminant history, or other local physicochemical properties. It also avoids some limitations of organic enrichment approaches, in which added organic matter may differ qualitatively from endogenous sediment organic matter and may create artificial physicochemical conditions for benthic fauna [45]. Because sediment granulometry can influence the movement and bioturbation effects of invertebrates, minimizing changes in grain-size structure strengthens the interpretation that differences among treatments were primarily associated with sediment [OM]. At the same time, our manipulation maintained the [OM] gradient within the range of spatial variation observed in Imboassica Lagoon [67,86], increasing the ecological relevance of the experimental conditions.
Some limitations should nevertheless be considered. First, the experiment lasted 48 h, which is appropriate for measuring short-term nutrient flux responses but may not capture longer-term changes in species interactions, sediment structure, microbial succession, or feedback between nutrient release and primary producers. Biodiversity effects can strengthen, weaken, or change direction over time as ecological interactions develop and as organisms modify their environment [60,61]. Second, our experiment manipulated sediment [OM] at the microcosm level, but did not incorporate fine-scale spatial heterogeneity within individual microcosms. In natural sediments, organisms encounter organic matter patches that vary over centimeters or less, and such microheterogeneity can influence foraging behavior, burrowing, and bioturbation intensity [45,97,108]. Third, we focused on NH3 flux as a key indicator of benthic–pelagic nutrient exchange, but bioturbation can simultaneously affect multiple processes, including oxygen consumption, phosphorus release, dissolved organic carbon flux, methane dynamics, microbial production, and organic matter processing [24,28,29,30,33,40,57,58,59,109]. Therefore, the degree to which sediment [OM] modulates biodiversity effects may differ among ecosystem processes.
Despite these limitations, our results have broader implications for understanding biodiversity effects in shallow aquatic ecosystems. Coastal lagoons and shallow lakes are systems in which benthic–pelagic coupling is often strong because the sediment surface is large relative to water volume and because biological activity in the sediment can rapidly influence water-column nutrient availability [22,52,64]. In such systems, changes in benthic biodiversity may alter not only local sediment processes but also nutrient availability for pelagic producers. Our findings indicate that losing bioturbator species may reduce NH3 fluxes, especially when assemblages are reduced from multispecies communities to single-species assemblages. At the same time, the consequences of biodiversity loss may depend on which species remain, because species identity strongly influenced fluxes in monocultures. Thus, biodiversity loss can affect benthic–pelagic nutrient exchange through both reductions in species richness and changes in functional identity.

5. Conclusions

Our study highlights the importance of considering multiple facets of biodiversity when evaluating ecosystem functioning in environmentally heterogeneous habitats. Species richness, identity, and composition are often treated as alternative or competing explanations for biodiversity effects, but our results show that they provide complementary information. Richness captured the overall saturating increase in NH3 fluxes from monocultures to multispecies assemblages, identity revealed strong differences among individual species, and composition suggested that differences among bicultures were weaker than differences among monocultures, at least under the conditions tested here. Sediment [OM] altered the magnitude of bioturbation-mediated fluxes but did not strongly modulate biodiversity effects through statistical interactions. Therefore, the functioning of benthic ecosystems appears to depend jointly on the environmental template provided by the sediment and on the biological structure of the bioturbator assemblage. We conclude that predicting benthic–pelagic nutrient exchange in shallow aquatic ecosystems requires integrating biodiversity facets with the trophic context of the sediment. Future studies should extend this approach to more complex natural communities and combine biodiversity manipulations with direct measurements of bioturbation intensity, bioirrigation, oxygen penetration, and microbial processes to better link biodiversity effects with the mechanisms operating in real lake ecosystems.

Author Contributions

Conceptualization, A.C.; methodology, A.C., L.S.C., J.J.F.L. and A.L.d.S.F.; software, A.C., L.S.C., R.D.G. and A.L.d.S.F.; validation, A.C., A.L.d.S.F. and J.J.F.L.; formal analysis, A.C., A.L.d.S.F. and L.S.C.; investigation, A.C., J.J.F.L., L.S.C. and A.L.d.S.F.; resources, F.d.A.E.; data curation, A.C. and L.S.C.; writing—original draft preparation, A.C. and A.L.d.S.F.; writing—review and editing, A.C., A.L.d.S.F., J.J.F.L., L.S.C. and F.d.A.E.; visualization, A.C., L.S.C. and A.L.d.S.F.; supervision, F.d.A.E. and J.J.F.L.; project administration, A.C. and F.d.A.E.; funding acquisition, A.C., R.D.G. and F.d.A.E. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by ongoing support from the Conselho Nacional de Desenvolvimento Científico e Tecnológico (CNPq) and the Fundação de Apoio ao Desenvolvimento do Ensino, Ciência e Tecnologia do Estado de Mato Grosso do Sul (FUNDECT), through research productivity grants awarded to A.C. (grant number 046362022-3) and R.D.G. (grant number 83026.8202024), respectively.

Data Availability Statement

Data used in this study will be made available upon reasonable request.

Acknowledgments

We are indebted to Fabricio Gonçalves and Francisco Brant for field and laboratory assistance.

Conflicts of Interest

The authors declare no conflicts of interest.

Abbreviations

The following abbreviations are used in this manuscript:
[OM]Organic matter concentration
TCTotal carbon
TNTotal nitrogen
TPTotal phosphorus

References

  1. Tilman, D. Causes, consequences and ethics of biodiversity. Nature 2000, 405, 208–211. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Balvanera, P.; Pfisterer, A.B.; Buchmann, N.; He, J.S.; Nakashizuka, T.; Raffaelli, D.; Schmid, B. Quantifying the evidence for biodiversity effects on ecosystem functioning and services. Ecol. Lett. 2006, 9, 1146–1156. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Cardinale, B.J.; Srivastava, D.S.; Duffy, J.E.; Wright, J.P.; Downing, A.L.; Sankaran, M.; Jouseau, C. Effects of biodiversity on the functioning of trophic groups and ecosystems. Nature 2006, 443, 989–992. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Hooper, D.U.; Adair, E.C.; Cardinale, B.J.; Byrnes, J.E.K.; Hungate, B.A.; Matulich, K.L.; Gonzalez, A.; Duffy, J.E.; Gamfeldt, L.; O’Connor, M.I. A global synthesis reveals biodiversity loss as a major driver of ecosystem change. Nature 2012, 486, 105–108. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Lefcheck, J.S.; Byrnes, J.E.K.; Isbell, F.; Gamfeldt, L.; Griffin, J.N.; Eisenhauer, N.; Hensel, M.J.S.; Hector, A.; Cardinale, B.J.; Duffy, J.E. Biodiversity enhances ecosystem multifunctionality across trophic levels and habitats. Nat. Commun. 2015, 6, 6936. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Duffy, J.E.; Godwin, C.M.; Cardinale, B.J. Biodiversity effects in the wild are common and as strong as key drivers of productivity. Nature 2017, 549, 261–264. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Huston, M.A. Hidden treatments in ecological experiments: Re-evaluating the ecosystem function of biodiversity. Oecologia 1997, 110, 449–460. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Loreau, M. Separating sampling and other effects in biodiversity experiments. Oikos 1998, 82, 600–602. [Google Scholar] [CrossRef] [Scilit]
  9. van der Plas, F. Biodiversity and ecosystem functioning in naturally assembled communities. Biol. Rev. 2019, 94, 1220–1245. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Cardinale, B.J.; Palmer, M.A.; Collins, S.L. Species diversity enhances ecosystem functioning through interspecific facilitation. Nature 2002, 415, 426–429. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Barry, K.E.; Mommer, L.; van Ruijven, J.; Wirth, C.; Wright, A.J.; Bai, Y.; Connolly, J.; De Deyn, G.B.; de Kroon, H.; Isbell, F.; et al. The future of complementarity: Disentangling causes from consequences. Trends Ecol. Evol. 2019, 34, 167–180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Caliman, A.; Pires, A.F.; Esteves, F.A.; Bozelli, R.L.; Farjalla, V.F. The prominence of and biases in biodiversity and ecosystem functioning research. Biodivers. Conserv. 2010, 19, 651–664. [Google Scholar] [CrossRef] [Scilit]
  13. Gonzalez, A.; Germain, R.M.; Srivastava, D.S.; Filotas, E.; Dee, L.E.; Gravel, D.; Thompson, P.L.; Isbell, F.; Wang, S.; Kéfi, S.; et al. Scaling-up biodiversity-ecosystem functioning research. Ecol. Lett. 2020, 23, 757–776. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Ricciardi, A.; Rasmussen, J.B. Extinction rates of North American freshwater fauna. Conserv. Biol. 1999, 13, 1220–1222. [Google Scholar] [CrossRef] [Scilit]
  15. Sala, O.E.; Chapin, F.S.; Armesto, J.J.; Berlow, E.; Bloomfield, J.; Dirzo, R.; Huber-Sanwald, E.; Huenneke, L.F.; Jackson, R.B.; Kinzig, A.; et al. Global biodiversity scenarios for the year 2100. Science 2000, 287, 1770–1774. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. Dudgeon, D.; Arthington, A.H.; Gessner, M.O.; Kawabata, Z.; Knowler, D.J.; Lévêque, C.; Naiman, R.J.; Prieur-Richard, A.H.; Soto, D.; Stiassny, M.L.; et al. Freshwater biodiversity: Importance, threats, status and conservation challenges. Biol. Rev. 2006, 81, 163–182. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Reid, A.J.; Carlson, A.K.; Creed, I.F.; Eliason, E.J.; Gell, P.A.; Johnson, P.T.J.; Kidd, K.A.; MacCormack, T.J.; Olden, J.D.; Ormerod, S.J.; et al. Emerging threats and persistent conservation challenges for freshwater biodiversity. Biol. Rev. 2019, 94, 849–873. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Giller, P.S.; Hillebrand, H.; Berninger, U.-G.; Gessner, M.O.; Hawkins, S.; Inchausti, P.; Inglis, C.; Leslie, H.; Malmqvist, B.; Monaghan, M.T.; et al. Biodiversity effects on ecosystem functioning: Emerging issues and their experimental test in aquatic environments. Oikos 2004, 104, 423–436. [Google Scholar] [CrossRef] [Scilit]
  19. Gamfeldt, L.; Hillebrand, H. Biodiversity effects on aquatic ecosystem functioning–maturation of a new paradigm. Int. Rev. Hydrobiol. 2008, 93, 550–564. [Google Scholar] [CrossRef] [Scilit]
  20. Gamfeldt, L.; Lefcheck, J.S.; Byrnes, J.E.K.; Cardinale, B.J.; Duffy, J.E.; Griffin, J.N. Marine biodiversity and ecosystem functioning: What’s known and what’s next? Oikos 2015, 124, 252–265. [Google Scholar] [CrossRef] [Scilit]
  21. Daam, M.A.; Teixeira, H.; Lillebø, A.I.; Nogueira, A.J.A. Establishing causal links between aquatic biodiversity and ecosystem functioning: Status and research needs. Sci. Total Environ. 2019, 656, 1145–1156. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Schindler, D.E.; Scheuerell, M.D. Habitat coupling in lake ecosystems. Oikos 2002, 98, 177–189. [Google Scholar] [CrossRef] [Scilit]
  23. Vaughn, C.C. Biodiversity losses and ecosystem function in freshwaters: Emerging conclusions and research directions. BioScience 2010, 60, 25–35. [Google Scholar] [CrossRef] [Scilit]
  24. Caliman, A.; Carneiro, L.S.; Leal, J.J.F.; Farjalla, V.F.; Bozelli, R.L.; Esteves, F.A. Community biomass and bottom up multivariate nutrient complementarity mediate the effects of bioturbator diversity on pelagic production. PLoS ONE 2012, 7, e44925. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  25. Chakraborty, A.; Saha, G.K.; Aditya, G. Macroinvertebrates as engineers for bioturbation in freshwater ecosystem. Environ. Sci. Pollut. Res. 2022, 29, 64447–64468. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Meysman, F.J.R.; Middelburg, J.J.; Heip, C.H.R. Bioturbation: A fresh look at Darwin’s last idea. Trends Ecol. Evol. 2006, 21, 688–695. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Queirós, A.M.; Birchenough, S.N.; Bremner, J.; Godbold, J.A.; Parker, R.E.; Romero-Ramirez, A.; Reiss, H.; Solan, M.; Somerfield, P.J.; Van Colen, C.; et al. A bioturbation classification of European marine infaunal invertebrates. Ecol. Evol. 2013, 3, 3958–3985. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  28. Figueiredo-Barros, M.P.; Caliman, A.; Leal, J.J.F.; Bozelli, R.L.; Farjalla, V.F.; Esteves, F.A. Benthic bioturbator enhances CH4 fluxes among aquatic compartments and atmosphere in experimental microcosms. Can. J. Fish. Aquat. Sci. 2009, 66, 1649–1657. [Google Scholar] [CrossRef] [Scilit]
  29. Caliman, A.; Carneiro, L.S.; Leal, J.J.F.; Farjalla, V.F.; Bozelli, R.L.; Esteves, F.A. Biodiversity effects of benthic ecosystem engineers on the spatial patterns of sediment CH4 concentration in an urban Neotropical coastal lagoon. Acta Limnol. Bras. 2013, 25, 302–314. [Google Scholar] [CrossRef] [Scilit]
  30. Booth, M.T.; Urbanic, M.; Wang, X.; Beaulieu, J.J. Bioturbation frequency alters methane emissions from reservoir sediments. Sci. Total Environ. 2021, 789, 148033. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Jones, C.G.; Lawton, J.H.; Shachak, M. Organisms as ecosystem engineers. Oikos 1994, 69, 373–386. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Mermillod-Blondin, F.; Rosenberg, R. Ecosystem engineering: The impact of bioturbation on biogeochemical processes in marine and freshwater benthic habitats. Aquat. Sci. 2006, 68, 434–442. [Google Scholar] [CrossRef] [Scilit]
  33. Caliman, A.; Carneiro, L.S.; Leal, J.J.F.; Farjalla, V.F.; Bozelli, R.L.; Esteves, F.A. Biodiversity effects of ecosystem engineers are stronger on more complex ecosystem processes. Ecology 2013, 94, 1977–1985. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Hölker, F.; Vanni, M.J.; Kuiper, J.J.; Meile, C.; Grossart, H.; Stief, P.; Adrian, R.; Lorke, A.; Dellwig, O.; Brand, A.; et al. Tube-dwelling invertebrates: Tiny ecosystem engineers have large effects in lake ecosystems. Ecol. Monogr. 2015, 85, 333–351. [Google Scholar] [CrossRef] [Scilit]
  35. Levin, L.; Boesch, D.; Covich, A.; Dahm, C.; Erséus, C.; Ewel, K.C.; Kneib, R.T.; Moldenke, A.; Palmer, M.A.; Weslawski, J.M.; et al. The function of marine critical transition zones and the importance of sediment biodiversity. Ecosystems 2001, 4, 430–451. [Google Scholar] [CrossRef] [Scilit]
  36. Snelgrove, P.V.R.; Blackburn, T.H.; Hutchings, P.A.; Alongi, D.M.; Grassle, J.F.; Hummel, H.; King, G.; Koike, I.; Lambshead, P.J.D.; Ramsing, N.B.; et al. The importance of marine sediment biodiversity in ecosystem processes. Ambio 1997, 26, 578–583. [Google Scholar]
  37. Gamfeldt, L.; Roger, F. Revisiting the biodiversity–ecosystem multifunctionality relationship. Nat. Ecol. Evol. 2017, 1, 0168. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Emmerson, M.; Solan, M.; Emes, C.; Paterson, D.M.; Raffaelli, D. Consistent patterns and the idiosyncratic effects of biodiversity in marine ecosystems. Nature 2001, 411, 73–77. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Solan, M.; Cardinale, B.J.; Downing, A.L.; Engelhardt, K.A.; Ruesink, J.L.; Srivastava, D.S. Extinction and ecosystem function in the marine benthos. Science 2004, 306, 1177–1180. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. Caliman, A.; Leal, J.J.F.; Esteves, F.A.; Carneiro, L.S.; Bozelli, R.L.; Farjalla, V.F. Functional bioturbator diversity enhances benthic–pelagic processes and properties in experimental microcosms. J. N. Am. Benthol. Soc. 2007, 26, 450–459. [Google Scholar] [CrossRef] [Scilit]
  41. Caliman, A.; Carneiro, L.S.; Santangelo, J.M.; Guariento, R.D.; Pires, A.P.; Suhett, A.L.; Quesado, L.B.; Scofield, V.; Fonte, E.S.; Lopes, P.M.; et al. Temporal coherence among tropical coastal lagoons: A search for patterns and mechanisms. Braz. J. Biol. 2010, 70, 803–814. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Jeong, Y.-H.; Choi, Y.-H.; Kwak, D.-H. Effect of benthic flux on the nutrient dynamics of bottom water during stratification in an artificial brackish lake. Water 2024, 16, 958. [Google Scholar] [CrossRef] [Scilit]
  43. Hiddink, J.G.; Wynter Davies, T.; Perkins, M.; Machairopoulou, M.; Neill, S.P. Context dependency of relationships between biodiversity and ecosystem functioning is different for multiple ecosystem functions. Oikos 2009, 118, 1892–1900. [Google Scholar] [CrossRef] [Scilit]
  44. Queirós, A.M.; Stephens, N.; Cook, R.; Ravaglioli, C.; Nunes, J.; Dashfield, S.; Harris, C.; Tilstone, G.H.; Fishwick, J.; Braeckman, U.; et al. Can benthic community structure be used to predict the process of bioturbation in real ecosystems? Prog. Oceanogr. 2015, 137, 559–569. [Google Scholar] [CrossRef] [Scilit]
  45. Bulling, M.T.; Solan, M.; Dyson, K.E.; Hernandez-Milian, G.; Luque, P.; Pierce, G.J.; Raffaelli, D.; Paterson, D.M.; White, P.C.L. Species effects on ecosystem processes are modified by faunal responses to habitat composition. Oecologia 2008, 158, 511–520. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Reich, P.; Knops, J.; Tilman, D.; Craine, J.; Ellsworth, D.; Tjoelker, M.; Lee, T.; Wedin, D.; Naeem, S.; Bahauddin, D.; et al. Plant diversity enhances ecosystem responses to elevated CO2 and nitrogen deposition. Nature 2001, 410, 809–812. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Fridley, J.D. Resource availability dominates and alters the relationship between species diversity and ecosystem productivity in experimental plant communities. Oecologia 2002, 132, 271–277. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  48. Zhang, Q.-G.; Zhang, D.-Y. Resource availability and biodiversity effects on the productivity, temporal variability and resistance of experimental algal communities. Oikos 2006, 114, 385–396. [Google Scholar] [CrossRef] [Scilit]
  49. Lewandowska, A.M.; Biermann, A.; Borer, E.T.; Cebrián-Piqueras, M.A.; Declerck, S.A.J.; De Meester, L.; Van Donk, E.; Gamfeldt, L.; Gruner, D.S.; Hagenah, N.; et al. The influence of balanced and imbalanced resource supply on biodiversity–functioning relationship across ecosystems. Philos. Trans. R. Soc. B 2016, 371, 20150283. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Godbold, J.A.; Bulling, M.T.; Solan, M. Habitat structure mediates biodiversity effects on ecosystem properties. Proc. R. Soc. B 2011, 278, 2510–2518. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  51. Søndergaard, M.; Larsen, S.E.; Johansson, L.S.; Lauridsen, T.L.; Jeppesen, E. Ecological classification of lakes: Uncertainty and the influence of year-to-year variability. Ecol. Indic. 2016, 61, 248–257. [Google Scholar] [CrossRef] [Scilit]
  52. Esteves, F.A.; Caliman, A. Águas continentais: Características do meio, compartimentos e suas comunidades. In Fundamentos de Limnologia, 3rd ed.; Esteves, F.A., Ed.; Editora Interciência: Rio de Janeiro, Brazil, 2011; pp. 113–118. [Google Scholar]
  53. Barko, J.W.; James, W.F. Effects of submerged aquatic macrophytes on nutrient dynamics, sedimentation, and resuspension. In The Structuring Role of Submerged Macrophytes in Lakes; Jeppesen, E., Søndergaard, M., Søndergaard, M., Christoffersen, K., Eds.; Springer: New York, NY, USA, 1998; Volume 131, pp. 197–214. [Google Scholar] [CrossRef] [Scilit]
  54. Marinho, C.C.; Meirelles-Pereira, F.; Gripp, A.R.; Guimarães, C.C.; Esteves, F.A.; Bozelli, R.L. Aquatic macrophytes drive sediment stoichiometry and the suspended particulate organic carbon composition of a tropical coastal lagoon. Acta Limnol. Bras. 2010, 22, 208–217. [Google Scholar] [CrossRef] [Scilit]
  55. Reynoldson, T.B.; Hamilton, H.R. Spatial heterogeneity in whole lake sediments—Towards a loading estimate. Hydrobiologia 1982, 91, 235–240. [Google Scholar] [CrossRef] [Scilit]
  56. Yang, C.; Yang, P.; Geng, J.; Yin, H.; Chen, K. Sediment internal nutrient loading in the most polluted area of a shallow eutrophic lake (Lake Chaohu, China) and its contribution to lake eutrophication. Environ. Pollut. 2020, 262, 114292. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  57. Leal, J.J.F.; Esteves, F.A.; Farjalla, V.F.; Enrich-Prast, A. Effect of Campsurus melanocephalus on NH4+, DOC fluxes, O2 uptake and bacterioplankton production in experimental microcosms with sediment-water interface of an Amazonian lake impacted by bauxite tailings. Int. Rev. Hydrobiol. 2003, 88, 167–178. [Google Scholar] [CrossRef] [Scilit]
  58. Nogaro, G.; Mermillod-Blondin, F.; Montuelle, B.; Boisson, J.-C.; Gibert, J. Chironomid larvae stimulate biogeochemical and microbial processes in a riverbed covered with fine sediment. Aquat. Sci. 2008, 70, 156–168. [Google Scholar] [CrossRef] [Scilit]
  59. Gautreau, E.; Volatier, L.; Nogaro, G.; Gouze, E.; Marmonier, P.; Mermillod-Blondin, F. Interactions between microbial activity and bioturbation modes of benthic invertebrates determine nutrient releases from reservoir sediments. Freshw. Biol. 2023, 68, 245–259. [Google Scholar] [CrossRef] [Scilit]
  60. Cardinale, B.J.; Ives, A.R.; Inchausti, P. Effects of species diversity on the primary productivity of ecosystems: Extending our spatial and temporal scales of inference. Oikos 2004, 104, 437–450. [Google Scholar] [CrossRef] [Scilit]
  61. Raffaelli, D. Biodiversity and ecosystem functioning: Issues of scale and trophic complexity. Mar. Ecol. Prog. Ser. 2006, 311, 285–294. [Google Scholar] [CrossRef] [Scilit]
  62. Chakraborty, A.; Saha, G.K.; Aditya, G. Interspecific interactions modulate bioturbation efficiency and nutrient dynamics in freshwater benthic communities. Sci. Rep. 2026, 16, 8679. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  63. Soffiati, A.A. Aspectos históricos das lagoas do norte do estado do Rio de Janeiro. In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); Esteves, F.A., Ed.; NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 1–38. [Google Scholar]
  64. Esteves, F.A.; Caliman, A.; Santangelo, J.M.; Guariento, R.D.; Farjalla, V.F.; Bozelli, R.L. Neotropical coastal lagoons: An appraisal of their biodiversity, functioning, threats and conservation management. Braz. J. Biol. 2008, 68, 967–981. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  65. Panosso, R.F.; Attayde, J.L.; Muehe, D. Morfometria das lagoas Imboassica, Cabiúnas, Comprida e Carapebus: Implicações para seu funcionamento e manejo. In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); Esteves, F.A., Ed.; NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 91–108. [Google Scholar]
  66. Esteves, F.A. (Ed.) Lagoa Imboassica: Impactos antrópicos, propostas mitigadoras e sua importância para a pesquisa ecológica. In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 401–429. [Google Scholar]
  67. Figueiredo-Barros, M.P.; Leal, J.J.F.; Esteves, F.A.; Rocha, A.M.; Bozelli, R.L. Life cycle, secondary production and nutrient stock in Heleobia australis (d’Orbigny 1835) (Gastropoda: Hydrobiidae) in a tropical coastal lagoon. Estuar. Coast. Shelf Sci. 2006, 69, 87–95. [Google Scholar] [CrossRef] [Scilit]
  68. Gonçalves, J.F., Jr.; Fonseca, J.J.L.; Callisto, M. Relações entre a composição granulométrica do sedimento e as comunidades de macroinvertebrados bentônicos nas lagoas Imboassica, Cabiúnas e Comprida (Macaé, RJ). In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); Esteves, F.A., Ed.; NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 299–310. [Google Scholar]
  69. Bozelli, R.L.; Caliman, A.; Guariento, R.D.; Carneiro, L.S.; Santangelo, J.M.; Figueiredo-Barros, M.P.; Leal, J.J.F.; Rocha, A.M.; Quesado, L.B.; Lopes, P.M.; et al. Interactive effects of environmental variability and human impacts on the long-term dynamics of an Amazonian floodplain lake and a South Atlantic coastal lagoon. Limnologica 2009, 39, 306–313. [Google Scholar] [CrossRef] [Scilit]
  70. Pereira, S.; Da-Silva, E. Descrição de uma nova espécie de Campsurus Eaton, 1868 do sudeste do Brasil, com notas biológicas (Ephemeroptera: Polymitarcyidae: Campsurinae). Rev. Bras. Biol. 1991, 51, 321–326. [Google Scholar]
  71. Gallepp, G.W. Chironomid influence on phosphorus release in sediment-water microcosms. Ecology 1979, 60, 547–556. [Google Scholar] [CrossRef] [Scilit]
  72. Leal, J.J.F.; Enrich-Prast, A.; Esteves, F.A.; Bozelli, R.; Farjalla, V.F. Influence of Campsurus melanocephalus bioturbation on oxygen profile and uptake in sediments of an Amazonian lake impacted by bauxite tailings. Arch. Hydrobiol. 2005, 162, 557–574. [Google Scholar] [CrossRef] [Scilit]
  73. Shaffer, P.L. Population ecology of Heteromastus filiformis (Polychaeta, Capitellidae). Neth. J. Sea Res. 1983, 17, 106–125. [Google Scholar] [CrossRef] [Scilit]
  74. Oeschger, R.; Vismann, B. Sulphide tolerance in Heteromastus filiformis (Polychaeta): Mitochondrial adaptations. Ophelia 1994, 40, 147–158. [Google Scholar] [CrossRef] [Scilit]
  75. Reise, K. Sediment mediated species interactions in coastal waters. J. Sea Res. 2002, 48, 127–141. [Google Scholar] [CrossRef] [Scilit]
  76. Rao, D.S. Ecology of Heteromastus similis Southern 1921 (Polychaeta: Capitellidae) in the Vasishta Godavari estuary. Proc. Anim. Sci. 1980, 89, 407–414. [Google Scholar] [CrossRef] [Scilit]
  77. Wild, C.; Roy, H.; Huettel, M. Role of pelletization in mineralization of fine-grained coastal sediments. Mar. Ecol. Prog. Ser. 2005, 291, 23–33. [Google Scholar] [CrossRef] [Scilit]
  78. Albertoni, E.F.; Palma-Silva, C.; Esteves, F.A. Macroinvertebrates associated with Chara in a tropical coastal lagoon (Imboassica lagoon, Rio de Janeiro, Brazil). Hydrobiologia 2001, 457, 215–224. [Google Scholar] [CrossRef] [Scilit]
  79. Ambühl, H.; Bührer, H. Zur Technik der Entnahme ungestörter Grossproben von Seesediment: Ein verbessertes Bohrlot. Schweiz. Z. Hydrol. 1975, 37, 175–186. [Google Scholar] [CrossRef] [Scilit]
  80. Callisto, M.; Gonçalves-Junior, J.F.; Leal, J.J.F.; Petrucio, M.M. Macroinvertebrados bentônicos nas lagoas Imboassica, Cabiúnas e Comprida. In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); Esteves, F.A., Ed.; NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 283–298. [Google Scholar]
  81. Solan, M.; Ward, E.R.; White, E.L.; Hibberd, E.E.; Cassidy, C.; Schuster, J.M.; Hale, R.; Godbold, J.A. Worldwide measurements of bioturbation intensity, ventilation rate, and the mixing depth of marine sediments. Sci. Data 2019, 6, 58. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  82. Jolliffe, P.A. The replacement series. J. Ecol. 2000, 88, 371–385. [Google Scholar] [CrossRef] [Scilit]
  83. Benedetti-Cecchi, L. Increasing accuracy of causal inference in experimental analyses of biodiversity. Funct. Ecol. 2004, 18, 761–768. [Google Scholar] [CrossRef] [Scilit]
  84. Allison, G.W. The implications of experimental design for biodiversity manipulations. Am. Nat. 1999, 153, 26–45. [Google Scholar] [CrossRef] [PubMed]
  85. Schmid, B.; Hector, A.; Huston, M.A.; Inchausti, P.; Nijs, I.; Leadley, P.W.; Tilman, D. The design and analysis of biodiversity experiments. In Biodiversity and Ecosystem Functioning: Synthesis and Perspectives; Loreau, M., Naeem, S., Inchausti, P., Eds.; Oxford University Press: New York, NY, USA, 2002; pp. 61–78. [Google Scholar]
  86. Petrucio, M.M.; Faria, B.M. Concentrações de carbono orgânico, nitrogênio total e fósforo disponível no sedimento das lagoas Cabiúnas e Comprida. In Ecologia das Lagoas Costeiras do Parque Nacional da Restinga de Jurubatiba e do Município de Macaé (RJ); Esteves, F.A., Ed.; NUPEM/UFRJ: Rio de Janeiro, Brazil, 1998; pp. 135–144. [Google Scholar]
  87. Stief, P.; Nazarova, L.; de Beer, D. Chimney construction by Chironomus riparius larvae in response to hypoxia: Microbial implications for freshwater sediments. J. N. Am. Benthol. Soc. 2005, 24, 858–871. [Google Scholar] [CrossRef] [Scilit]
  88. Koroleff, F. Determination of ammonia. In Methods of Sea Water Analysis; Grasshoff, K., Ehrhardt, M., Kremling, K., Eds.; Verlag Chemie: Weinheim, Germany, 1978; pp. 151–157. [Google Scholar]
  89. Jackson, M.L. Soil Chemical Analysis; Prentice-Hall: Englewood Cliffs, NJ, USA, 1962. [Google Scholar]
  90. Cardinale, B.J.; Nelson, K.; Palmer, M.A. Linking species diversity to the functioning of ecosystems: On the importance of environmental context. Oikos 2000, 91, 175–183. [Google Scholar] [CrossRef] [Scilit]
  91. Cardinale, B.J.; Palmer, M.A. Disturbance moderates biodiversity-ecosystem function relationships: Experimental evidence from caddisflies in stream mesocosms. Ecology 2002, 83, 1915–1927. [Google Scholar] [CrossRef] [Scilit]
  92. Cardinale, B.J.; Weis, J.J.; Forbes, A.E.; Tilmon, K.J.; Ives, A.R. Biodiversity as both a cause and consequence of resource availability: A study of reciprocal causality in a predator-prey system. J. Anim. Ecol. 2006, 75, 497–505. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  93. Biles, C.L.; Solan, M.; Isaksson, I.; Paterson, D.M.; Emes, C.; Raffaelli, D.G. Flow modifies the effect of biodiversity on ecosystem functioning: An in situ study of estuarine sediments. J. Exp. Mar. Biol. Ecol. 2003, 285–286, 165–177. [Google Scholar] [CrossRef] [Scilit]
  94. Caliman, A.; Carneiro, L.S.; Bozelli, R.L.; Farjalla, V.F.; Esteves, F.A. Bioturbating space enhances the effects of non-additive interactions among benthic ecosystem engineers on cross-habitat nutrient regeneration. Oikos 2011, 120, 1639–1648. [Google Scholar] [CrossRef] [Scilit]
  95. Duffy, J.E.; Cardinale, B.J.; France, K.E.; McIntyre, P.B.; Thébault, E.; Loreau, M. The functional role of biodiversity in ecosystems: Incorporating trophic complexity. Ecol. Lett. 2007, 10, 522–538. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  96. Godbold, J.A.; Solan, M. Relative importance of biodiversity and the abiotic environment in mediating an ecosystem process. Mar. Ecol. Prog. Ser. 2009, 396, 273–282. [Google Scholar] [CrossRef] [Scilit]
  97. Griffin, J.N.; Jenkins, S.R.; Gamfeldt, L.; Jones, D.; Hawkins, S.J.; Thompson, R.C. Spatial heterogeneity increases the importance of species richness for an ecosystem process. Oikos 2009, 118, 1335–1342. [Google Scholar] [CrossRef] [Scilit]
  98. Ieno, E.N.; Solan, M.; Batty, P.; Pierce, G.J. How biodiversity affects ecosystem functioning: Roles of infaunal species richness, identity and density in the marine benthos. Mar. Ecol. Prog. Ser. 2006, 311, 263–271. [Google Scholar] [CrossRef] [Scilit]
  99. Mermillod-Blondin, F.; François-Carcaillet, F.; Rosenberg, R. Biodiversity of benthic invertebrates and organic matter processing in shallow marine sediments: An experimental study. J. Exp. Mar. Biol. Ecol. 2005, 315, 187–209. [Google Scholar] [CrossRef] [Scilit]
  100. Norling, K.; Rosenberg, R.; Hulth, S.; Grémare, A.; Bonsdorff, E. Importance of functional biodiversity and species-specific traits of benthic fauna for ecosystem functions in marine sediment. Mar. Ecol. Prog. Ser. 2007, 332, 11–23. [Google Scholar] [CrossRef] [Scilit]
  101. Solan, M.; Batty, P.; Bulling, M.T.; Godbold, J.A. How biodiversity affects ecosystem processes: Implications for ecological revolutions and benthic ecosystem function. Aquat. Biol. 2008, 2, 289–301. [Google Scholar] [CrossRef] [Scilit]
  102. Braeckman, U.; Provoost, P.; Gribsholt, B.; Van Gansbeke, D.; Middelburg, J.J.; Soetaert, K.; Vincx, M.; Vanaverbeke, J. Role of macrofauna functional traits and density in biogeochemical fluxes and bioturbation. Mar. Ecol. Prog. Ser. 2010, 399, 173–186. [Google Scholar] [CrossRef] [Scilit]
  103. Needham, H.R.; Pilditch, C.A.; Lohrer, A.M.; Thrush, S.F. Habitat dependence in the functional traits of Austrohelice crassa, a key bioturbating species. Mar. Ecol. Prog. Ser. 2010, 414, 179–193. [Google Scholar] [CrossRef] [Scilit]
  104. Needham, H.R.; Pilditch, C.A.; Lohrer, A.M.; Thrush, S.F. Context-specific bioturbation mediates changes to ecosystem functioning. Ecosystems 2011, 14, 1096–1109. [Google Scholar] [CrossRef] [Scilit]
  105. Hale, R.; Mavrogordato, M.N.; Tolhurst, T.J.; Solan, M. Characterizations of how species mediate ecosystem properties require more comprehensive functional effect descriptors. Sci. Rep. 2014, 4, 6463. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  106. Wohlgemuth, D.; Solan, M.; Godbold, J.A. Species contributions to ecosystem process and function can be population dependent and modified by biotic and abiotic setting. Proc. R. Soc. B Biol. Sci. 2017, 284, 20162805. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  107. Dolbeth, M.; Crespo, D.; Leston, S.; Solan, M. Realistic scenarios of environmental disturbance lead to functionally important changes in benthic species-environment interactions. Mar. Environ. Res. 2019, 150, 104770. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  108. Dyson, K.E.; Bulling, M.T.; Solan, M.; Hernandez-Milian, G.; Raffaelli, D.G.; White, P.C.L.; Paterson, D.M. Influence of macrofaunal assemblages and environmental heterogeneity on microphytobenthic production in experimental systems. Proc. R. Soc. B Biol. Sci. 2007, 274, 2547–2554. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  109. Mermillod-Blondin, F. The functional significance of bioturbation and biodeposition on biogeochemical processes at the water-sediment interface in freshwater and marine ecosystems. J. N. Am. Benthol. Soc. 2011, 30, 770–778. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Bioturbation-mediated NH3 flux as a function of bioturbator species richness (mono-, bi-, and tricultures) across sediment trophic status (Low, Medium, and High organic matter concentrations). Bioturbation-mediated fluxes were calculated by subtracting the mean NH3 flux of sediment-only controls from the flux observed in each fauna-containing microcosm within the same sediment trophic status level. For each sediment trophic status level, one-species treatments correspond to the mean of all monocultures (three species × three replicates; total n = 9), two-species treatments correspond to the mean of all bicultures (three pairwise species combinations × three replicates; total n = 9), and three-species treatments correspond to the triculture treatment (one three-species combination × nine replicates; total n = 9). Error bars represent standard errors. Different letters above bars indicate significant statistical differences of NH3 flux among species richness levels within each sediment trophic status level (p < 0.05; Tukey post hoc test).
Limnolrev 26 00039 g001
Figure 2. Bioturbation-mediated NH3 flux as a function of (A) species identity and (B) species composition across different sediment trophic states (Low, Medium, and High). Bioturbation-mediated fluxes were calculated by subtracting the mean NH3 flux of sediment-only controls from the flux observed in each fauna-containing microcosm within the same sediment trophic status level. In (A), colors represent the three species used in monoculture treatments, with each bar representing the mean of one species monoculture within a given sediment trophic status level (three replicates per bar). In panel (B), diagonally striped bars represent pairwise species combinations using the same colors assigned to the corresponding species in panel A, with each bar representing the mean of one biculture composition within a given sediment trophic status level (three replicates per bar). Error bars represent standard errors. In (A), different letters above bars indicate significant statistical differences of NH3 flux among species identities within each sediment trophic status level (p < 0.05; Tukey post hoc test). In (B), different letters above brackets indicate significant statistical differences of NH3 flux among sediment trophic status levels, irrespective of species composition (p < 0.05; Tukey post hoc test). Species name abbreviations are Cm = C. melanocephalus; Ha = H. australis and Hs = H. similis.
Limnolrev 26 00039 g002
Table 1. Mean ± standard deviation (n = 3) of sediment organic matter, total carbon, total nitrogen, and total phosphorus contents across the three experimental * sediment trophic status levels (High, Medium and Low). All values are expressed as percentages of sediment dry weight.
VariableHighMediumLow
Organic matter10.03 ± 0.424.48 ± 0.262.61 ± 0.12
Total carbon2.65 ± 0.211.07 ± 0.090.33 ± 0.02
Total nitrogen0.25 ± 0.0120.13 ± 0.0070.07 ± 0.003
Total phosphorus0.053 ± 0.0030.029 ± 0.0010.013 ± 0.001
* The High trophic status corresponds to unaltered natural sediment, whereas the Medium and Low trophic status levels correspond to sediments diluted with 50% and 75% organic matter-free mineral sediment on a dry-weight basis, respectively.
Table 2. Summary of the factorial analysis of variance testing the individual and interactive effects of sediment trophic status and bioturbator species richness on NH3 flux across the sediment–water interface. df and MS represent degrees of freedom and mean squares, respectively. * Indicates significant statistical effects (p < 0.05).
Source of VariationDfMSFp
Intercept1289.95227,186.57<0.0001 *
Trophic status (TS)20.1079.990.0001 *
Richness (R)20.0948.780.0004 *
TS × R40.0040.330.85
Error720.011
Table 3. Summary of the factorial analysis of variance testing the individual and interactive effects of sediment trophic status with (a) bioturbator species identity and (b) bioturbator species composition on NH3 flux across the sediment–water interface. Species identity and composition were tested by comparing species monocultures and bicultures within their respective species richness levels. df and MS represent degrees of freedom and mean squares, respectively. * Indicates significant statistical effects (p < 0.05).
Source of VariationdfMSFp
(a)
Species monocultures
Intercept189.8378427.65<0.0001 *
Trophic status (TS)20.0242.240.14
Species identity (SI)20.13112.300.0004 *
TS × SI40.0020.230.91
Error180.011
(b)
Species bicultures
Intercept1100.48320,861.32<0.0001 *
Trophic status (TS)20.04810.030.001 *
Species composition (SC)20.0173.500.052
TS × SC40.0071.500.243
Error180.005
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.