


Abstract
Microbial fuel cells (MFC) are an emerging technology for waste, wastewater and polluted soil treatment. In this manuscript, pollutants that can be treated using MFC systems producing energy are presented. Furthermore, the applicability of MFC in environmental monitoring is described. Common microbial species used, release of genome sequences, and gene regulation mechanisms, are discussed. However, although scaling-up is the key to improving MFC systems, it is still a difficult challenge. Mathematical models for MFCs are used for their design, control and optimization. Such models representing the system are presented here. In such comprehensive models, microbial growth kinetic approaches are essential to designing and predicting a biosystem. The empirical and unstructured Monod and Monod-type models, which are traditionally used, are also described here. Understanding and modelling of the gene regulatory network could be a solution for enhancing knowledge and designing more efficient MFC processes, useful for scaling it up. An advanced bio-based modelling concept connecting gene regulation modelling of specific metabolic pathways to microbial growth kinetic models is presented here; it enables a more accurate prediction and estimation of substrate biodegradation, microbial growth kinetics, and necessary gene and enzyme expression. The gene and enzyme expression prediction can also be used in synthetic and systems biology for process optimization. Moreover, various MFC applications as a bioreactor and bioremediator, and in soil pollutant removal and monitoring, are explored.
1. Introduction
Microbial fuel cells (MFCs) are a promising technology in the field of bioelectrochemical systems and an emerging research field for toxic and persistent pollutant degradation, power generation, fuel and chemical production [1,2]. Many studies on MFC systems have focused on MFC laboratory-scale reactors. However, scaling up is a crucial challenge for advances in the technology and development in the field of industrial bioelectrochemical processes.
Mathematical modeling plays a significant role in expanding our knowledge of MFC reactors, by recognizing the leading factors in pollutant biodegradation and power generation, and can provide guidelines for scale-up strategies [3]. Kinetic models are used for predicting, optimizing and controlling bioprocesses, and bioreactor design. These models are categorized as segregated, unsegregated, structured and unstructured. The unsegregated and segregated models vary in how the cell properties in the bioprocess are considered [4]. The structured models study specific intracellular reactions, which involve components, such as DNA, RNA or proteins. The unstructured models consider the cell a black box and model the death and growth of microbes. The description and prediction of microbial growth and substrate biodegradation kinetics is significant for the prediction of the bioprocess performance and the fate of organic pollutants in natural and engineered biosystems.
Common microbial growth kinetic models in MFCs are the Monod [5] and Monod-type kinetics. For instance, Zhang et al. [6] predicted substrate degradation kinetics in a dual-chamber MFC using four different Monod-type kinetic models. In this study one can note that nitrate degradation was not predicted well by most of the models, giving coefficients of determination (R2) between 0.82 and 0.98. In another study [7], substrate degradation was predicted using Monod kinetics without using different experimental sets to validate the model. Furthermore, upon use of different microorganisms, in an attempt to enhance power density, Mirolieu et al. [8] used Moser and Monod models to predict the specific growth rate and, also, in their case, the R2 was not that high, ranging from 0.8 to 0.92.
Monod-type models employ unstructured kinetics, are empirical and assume the existence of a single metabolic reaction that follows Michaelis–Menten kinetics and is responsible for substrate uptake. They may also assume a substrate inhibition effect or the existence of several substrates. Typically, these models cannot describe or predict the performance of a biosystem in larger than laboratory-scale operations [9]. Models developed based on Monod expressions often fail to predict experiments based on model-based control and optimization and have narrow applicability. Furthermore, these models do not consider the effect of the dynamic microbial metabolism and disregard transcriptional regulation [10]. However, thanks to transcriptional regulation, the metabolic networks are activated by initiating the relevant metabolic cascades for substrate biotransformation, Krebs cycle activation, and, hence, microbial growth [11]. In current MFC mathematical modelling approaches, the use of such empirical and unstructured models is a limiting factor for scaling up. Mechanistic insight is essential for optimization and accurate bioprocess design. The existing models, therefore, need to be upgraded in the near future and development of new mathematical modeling approaches accounting for gene regulation is essential for understanding and addressing the challenges of industrialization [12].
An advanced mathematical modeling approach is presented here based on the Tsipa et al. [11] microbial growth kinetics model, which was coupled to gene regulation of the main activated metabolic pathway for mixed substrates biodegradation. The main gene regulatory network responsible for substrate biodegradation and microbial growth was designed and modelled. Transcriptional kinetics was used to tune the model. This model was then combined with the microbial growth kinetic model and validated by using different experimental data sets. The gene regulatory-microbial growth kinetic model was used for model-based optimization of the bioprocess through knowledge of the molecular elements which play a significant role in the regulation of substrate biotransformation metabolism. Control, optimization and, thus, potentially scaling-up of the MFC process may therefore be achievable through regulatory network modelling. Furthermore, the goals of the study are to: (i) highlight the MFC broad applicability, (ii) present the most common microorganisms used in MFCs, (iii) show the level of genomic insights on the microbes used, (iv) describe the most common mathematical modelling approaches, and microbial growth kinetics models used in MFCs, while (v) explaining the advanced mathematical modeling approach.
2. Microbial Fuel Cells (MFCs) as a Depollution System for Recalcitrant Pollutants and Specific Pollutants
MFCs are a promising technology that can act as a depollution system for wastewater and polluted soil. The pollution in wastewater and soil can happen due to the presence of organic (e.g. polychlorinated biphenyls (PCB), dichlorodiphenyl-dichloroethylene (DDE)) or inorganic contaminants (e.g., metals). Metals are natural components of ecosystems [13] but at the same time they are the most dangerous type of environmental pollutant [13]. Heavy metals are released mostly from anthropogenic sources, such as mining, metallurgy, batteries, electroplating, electrolysis, tanneries, pesticides and fertilizers. The removal of specific pollutants such as heavy metals with MFCs is a growing field of study [13]. A survey of microbial fuel cells as depollution systems for heavy metal pollution and specific pollution such as DDE is presented here. Other organic matter depollution through MFC systems has recently been thoroughly reviewed. Recalcitrant compounds which have been studied are monoaromatic [14] and polyaromatic [15] hydrocarbons (MAHs and PAHs), antibiotics, synthetic dyes, nitrogen-containing organic compounds, ethyl acetate, pesticides, sulfur-containing compounds and emerging contaminants [16].
Heavy metals include lead (Pb), chromium (Cr), arsenic (As), zinc (Zn), cadmium (Cd), copper (Cu), mercury (Hg), nickel (Ni), iron (Fe), and precious metals such as silver, gold, and platinum. The light metals, such as magnesium, aluminum and titanium, were discovered in 1809 together with other heavy metals like gallium, thallium and hafnium. The heavy metal removal is performed in terms of their reduction-oxidation and production of less toxic forms, such as in the case of Cr(VI) to Cr(III). Among heavy metal ions, Cu, Hg, Cr, Cd and Pb bioaccumulate through the food chain, rather than degrade into harmless products [13], and they are highly dangerous for living organisms [13,17].
Coupling microbial fuel cells with other techniques such as phytoremediation [18], electrokinetics, microbial electrolysis cells and the use of microalgae can effectively improve the depollution and energy conversion performance of a system.
In 2020, Zhang et al. [19] affirmed that the migration of soil heavy metals is mainly based on the electricity generation of MFCs, and the migration efficiency of heavy metals in soil increased with increasing electricity generation. They found that HCl was the most suitable auxiliary reagent for the removal of heavy metals from soil with MFCs in terms of electricity generation performance, the efficient removal of heavy metals and decrease in heavy metals in the cathode.
2.1. Copper (Cu)
The removal efficiency of acid-soluble Cu from the soil near the anode was found by Zhang et al. [19]. The removal reached 42.5% after 63 days of operation at an external resistance of 100 Ω and electrode spacing of 10 cm, and Cu2+ in the cathode was completely removed within 21 days. This result was achieved with a three-chamber microbial fuel cell that avoided the adverse effects of H+ diffusion on anode microorganisms in the acidic cathode and the precipitation of heavy metals in the soil close the cathode (S4), while also achieving migration of copper from the soil and reduction of Cu2+ in the catholyte.
2.2. Chromium (Cr)
The hexavalent chromium Cr(VI) and trivalent chromium Cr(III) are the main valence states of chromium in the natural environment. Cr(VI) is water soluble with high toxicity in the full pH range, while Cr(III), being less mobile, is less toxic and tends to form Cr(OH)3 precipitates. Li et al. [20] found that MFCs operated in two-chambers are able to reduce Cr(VI) to non-toxic Cr(III) using three different cathode materials such as carbon cloth, carbon brush and carbon felt. They also reported that 80 mg/L Cr(VI) was completely removed by MFCs with a carbon cloth cathode in 72 h at an optimized pH of 2 while only 33.45% and 12.72% of Cr(VI) removal efficiency were obtained using carbon brush and carbon felt, respectively, as cathode materials.
In 2019, Zhang et al. [21] developed a reactor combining adsorption and microbial fuel cells using Platanus acerifolia for removing Cr(VI) from groundwater and soils, where the initial Cr(VI) concentration was 50 mg/L and the adsorption efficiency achieved 98% after 16 h. The overall Cr(VI) removal efficiency was significantly improved through leaching and 40% of the Cr(VI) in the soil column was removed.
In 2020, Ali et al. [22] reached a maximum power density of 154 mW/m2 and a high Cr(VI) removal efficiency (100%) with a dual-chamber MFC where the catholyte concentration was 15 mg/L. FeS@rGO nanocomposites synthesized with a facile precipitation method were used to decorate the graphite felt cathode. The modified cathode was found to be better at synergistic Cr(VI) reduction and electricity generation. Electrochemical characterisation revealed that the enhanced performance was due to the excellent conductivity, low internal resistance and improved electrochemical performance of FeS@rGO nanocomposites. Furthermore, it was observed that rapid Cr(VI) reduction has a positive influence on the COD removal efficiency and electrogenic activity in the anode.
2.3. Lead (Pb) and Zinc (Zn)
Coupled remediation techniques may improve metal removal efficiency and rates, thus reinforcing their application in soil remediation. In 2016, an electrokinetic remediation for toxic metal contaminated soil driven by microbial fuel cells was presented [23]. It was verified that electricity recovered from MFCs could power electrokinetic remediation effectively. Moreover, the metal removal efficiency and its influence on soil physiological properties were investigated. The metal reduction is possible through oxidation of organic substances in soils by microorganisms, producing energy and in this process metals migrate from anode to cathode region. The concentrations of Cd and Pb in the soils increased gradually through the anode to the cathode regions after remediation. After about 143 and 108 days, a removal efficiency of 31.0% and 44.1% in the anode region was achieved for Cd and Pb, respectively.
In 2018, Song et al. [24] provided other case studies of coupling microbial fuel cell and electrokinetic remediation for Pb and Zn in contaminated soil. The effects of adding wheat straw in soil/terrestrial MFCs was also analysed. Adding straw enhanced the substrate mass transfer in the anode region, improving the electric output, which was able to promote Pb and Zn migration in the soil. In fact, the electrical performance of the MFCs was influenced by the amount of straw added. The soil MFC with 3% straw added improved Pb removal efficiency from 15% to 37.2%, and Zn removal efficiency from 7.3% to 15.1%, and the electricity produced increased from 10.5 to 25.7 mW m−2, if compared to a soil MFC without straw added.
2.4. Cadmium (Cd)
Cadmium is usually present in wastewater rather than in soil. In 2014 Abourached et al. [25] investigated the effects of cadmium and zinc concentrations on the power conversion of a single-chamber air-cathode MFC and its depollution capabilities. The results reported high power generation (3.6 W/m) and high Cd (90%) and Zn (97%) removal efficiency. Moreover, it was found that the Cd maximum tolerable concentration for electrochemically active microorganisms was 200 mM and 400 mM for Zn. In fact, increasing the concentrations of Cd to 300 mM and Zn to 500 mM resulted in voltage drops of 71% and 74%, respectively. They reported that biosorption and sulfide precipitation are the major mechanisms for heavy metal removal in MFCs.
Microbial electrolysis cells (MECs) needing an external energy supply can be coupled with MFCs as potential bio-electrochemical technologies for reducing heavy metals such as Cd (II) [26]. Choi et al. [27] analyzed a Cd (II)-MEC coupled with a Cr(VI)-MFC to recover Cd (II). The Cr(VI)-MFC could provide the external source supply for the Cd(II)-MEC system. It was observed that after 60 h of reaction, the 200 ppm Cr(VI) and 50 ppm Cd(II) removal efficiencies were 13.95% ±0.73% and 93.43% ±0.17%, respectively. Furthermore Pb(II)-MEC connected with Cr(VI)-MFC are capable of simultaneously reducing Cr(VI) and Pb(II) without external energy input [28].
In 2018, microalgae (Chlorella sp. QB-102) were introduced into an MFC as the cathode for Cd(II) removal using nickel foam/graphene as electrodes [29]. It was found that graphene enhanced power generation and decreased the internal resistance and start-up time in the algal-cathode MFC. Graphene further improved the maximum tolerable concentrations of Cd(II) in the algal-cathode, which was estimated to be 50 ppm. Using nickel foam/graphene electrodes, the algal-cathode MFC achieved a Cd(II) removal efficiency of almost 95% and a maximum adsorption amount of 115 g/m2. It was found that hydroxide precipitation and biosorption are the major mechanisms for Cd removal in a biocathode self-sustained MFC.
2.5. Dichlorodiphenyl-Dichloroethylene (DDE)
In 2020, a case study of MFCs using soil contaminated with DDE (2,2-bis (dichlorodiphenyl-dichloroethylene or p-chlorophenyl)-1,1-dichloroetylene), a persistent metabolite of the DDT (dichlorodiphenyl-trichloroethane) pesticide, was conducted to analyse the cell characteristics and the effectiveness in removing soil contamination by a persistent organic pollutant [30,31]. MFCs have been tested for triggering and promoting DDE degradation by stimulating exo-electrogen microorganisms that catalyse oxidation and reduction reactions in two electrodes. At 2 months into the experiment, MFCs promoted a significant pollutant degradation (39%), if compared to the their absence. Moreover, adding organic carbon (compost) stimulated microbial activity and improved the MFC performance.
3. Pure and Mixed Microbial Cultures in MFC Systems
The Geobacter and Shewanella species are well known electron donors which have been widely used in bioelectrochemical systems in various applications. Several microorganisms have been discovered over the years that are able to produce electrons via various directly or indirectly electron transport pathways. In Table 1, microorganisms used in MFC systems are presented. For each microorganism, the extracellular electron transport pathway is shown together with the configuration of the MFC and, if applicable, the substrates used.
Table 1.
Microorganisms used in microbial fuel cell (MFC) systems for their extracellular electron transport mechanisms.
Some of these microorganisms have been genetically engineered to provide better results in terms of current added-value compounds production, sustainable microbial growth and power generation compared to the wild-type strains [32,33]. A limited use of algae in microbial fuel cells has also been reported in a few studies.
4. Release of Genome Sequence and Gene Regulatory Mechanisms Related to Substrate(s) Biodegradation in MFCs
Acetate, glucose, glycerol, nitrate, propionate, fumarate and lactate have been widely used in MFC systems as substrates [100]. Knowledge about the gene regulation and metabolic steps involved in biotransformation of such substrates has increased significantly over recent decades, as explained below. MFCs are effectively used for removal of the recalcitrant pollutants contained in waste, wastewater and polluted soil. Genomic insights and knowledge of the gene regulatory mechanisms involved in the biotransformation of such metabolic pathways will be a key step towards control and optimization of the process through gene regulation modelling.
Extracellular electron transport pathways are of great significance in bioelectrochemical systems as they represent their essential operational principle. Gene regulation related to these pathways has been widely explored, revealing the genes, enzymes and pathways of electron transportation (e.g., [101]), as shown in Table 1. One of the factors which also affect MFC performance to a high extent is the fate of substrate biodegradation, which results in Krebs cycle activation and, potentially, microbial growth. However, gene regulation related to substrate degradation has not been adequately explored yet.
The most common method used to estimate substrate degradation is COD reduction during MFC operation [7]. The biosystem is thus considered a black box, while understanding of the biochemical and genetic mechanisms involved is not possible. As the Geobacter and Shewanella species have been traditionally used in MFCs, it is the gene regulation mechanisms of different strains of these species that have been discovered. For instance, after discovery of the genome sequence of Geobacter metallireducens, the metabolic pathways and gene regulation of acetate, butyrate, propionate, pyruvate, oxaloacetate, phosphoenolpyruvate, fumarate and nitrate fate towards microbial growth were found [102]. Furthermore, release of the G. sulfurreducens genome sequence has led to many studies in gene regulation and metabolism of different substrates. Similarly, the genome sequence of Shewanella odeinsis [103] allowed the determination of the intermediary metabolic steps of glycolysis, Krebs cycle, glyoxalate bypass, the pentose phosphate and the Entner–Doudoroff pathways, together with the metabolic pathways of several substrates such as propionate, glycerol, formate, pyruvate, lactate, acetate and ethanol [104].
In many cases, glycolysis accounts for the substrate biotransformation metabolic pathway because microbes utilize organic compounds to grow [80]. However, glucose and glucose-related substrates are not considered pollutants and their pathways cannot be a general representation of substrate biotransformation in MFCs. Only a few studies have until now revealed recalcitrant pollutants biotransformation metabolism, such as Hassan et al. [1], who traced the metabolic pathways of chlorophenol under aerobic and anaerobic conditions. More research in this direction is, therefore, necessary.
The genomes of different strains of Pseudomonas aeruginosa and Escherichia coli have been sequenced, allowing us to understand several gene regulation mechanisms in the metabolic pathways of recalcitrant pollutants. Similarly, genomic insights into other microorganisms which happen to be also used in MFC systems have been explored. This knowledge can be combined with and connected to their use in MFC systems to enhance our knowledge about gene regulation and the metabolic pathways of substrate biotransformation in MFCs. Information regarding gene regulation mechanisms can assist in accurate mathematical modelling to predict microbial growth kinetics as explained below. Modeling of gene regulation can lead to model-based gene control to increase substrate biodegradation, biomass growth, product formation or electricity production, which is also explained below. Furthermore, this information can be used in genome engineering to overexpress or knock out genes in order to increase substrate biodegradation, electrons availability, biomass growth etc. This information can also be used in synthetic biology to engineer the cells and systems biology to predict behavior and phenotypes.
5. Comprehensive Mathematical Models to Predict MFC Output
The complexity of an MFC system can be simplified when expressed in a mathematical model using a combined electrochemical and microbial growth kinetic approach, although it should be validated with experimental data [3]. A mathematical model of an MFC system involves the effects of biological, design and operational parameters. Biological parameters may include microbial culture information such as microbial growth, substrate biodegradation kinetics, extracellular electron transfer mechanism and source of microorganisms; design parameters may include membrane characteristics, electrode material, configuration of the MFC and volume of the chamber; operational parameters may include continuous, batch and fed-batch systems, flow rate, pH, temperature, feed concentration, current applied or potential and external resistance [12,105,106,107]. These parameters are related to the MFC system variables which are the outputs of the model. Furthermore, a mathematical model of an MFC system can be built while considering either (i) pure or mixed microbial cultures, (ii) the mode of transportation of the extracellular electron transfer pathway (i.e., direct or indirect transportation), or (iii) biofilm formation [105].
In addition, mathematical model strategies encompass engineering-based models [105], statistical models, black box models, electrochemical simulation, biological approach models, conceptual models, sensitivity analysis and polarization model [3]. Another difference among MFC mathematical models is whether they are anode-based or anode/cathode models [108].
This paper focuses on engineering-based approaches. Dynamic or steady-state models are typically developed by using either ordinary differential equations (ODE) or partial differential equations (PDE). Among them, models developed with ODEs are dependent on time without accounting for spatial dimension, and they are formulated in a simple way resulting in a relatively low computation time and cost. On the other hand, models developed with PDEs consider both time and spatial resolutions, leading to a more instructive and complete approach. However, both computational time and cost are moderately greater compared to ODE models [105]. Furthermore, some models assume steady state conditions accounting for one spatial dimension [12]. The choice of model equations is based on the expected model performance and, most importantly, the application. In Table 2, the most well-known dynamic and steady state mathematical models of MFCs are presented.
Table 2.
MFC mathematical modelling approaches (from models, control, optimization); ODE and PDE: ordinary and partial differential equations.
Although mathematical modelling of MFCs is not as developed as in other scientific fields, over recent years several review papers have attempted to gather the different mathematical models developed and the different mathematical modelling strategies. As observed in Table 2, the dynamic models typically use Monod-type equations to predict substrate biodegradation kinetics and microbial growth, ignoring the gene regulation governing the process. Briefly, the most important models are explained below.
Zhang and Halme [109] suggested one of the first comprehensive studies in mathematical modeling of MFCs. The model was developed using ordinary differential equations (ODE) and is considered a reference point for the advanced models developed in later years. In this model, Monod kinetics are used to represent the substrate biodegradation fate. The MFC used was a dual chamber one.
A more comprehensive model than that of Zhang and Halme was developed by Picioreanu et al. [110]. The model was developed using ODEs in a dual-chamber MFC operating in batch mode, accounting for the phenomena in the anode. The substrate used was acetate and the microorganism modelled was G. sulfurreducens as a microorganism culture. Acetate biodegradation and microbial growth are represented by a Monod kinetics model.
Zeng et al. [111] developed a mathematical model of a dual-chamber MFC considering both anode and cathode factors with a microbial consortium. Two different substrates are used in the anode: acetate and glucose-glutamic acid. Mathematical expressions of Monod kinetics are used to model the mass balances of substrates and microbial growth. This model has been used to guide the performance of experiments and as a reference point for dual-chamber models.
Pinto et al. [112] developed a mathematical model using ODEs of the anode of a single-chamber MFC. Two different microbial species were considered (methanogenic and anodophilic bacteria). Mass balances of substrate degradation, species growth and mediator are expressed using Monod kinetics. The parameters of the model are estimated by applying the Neder–Mead simplex algorithm. This model can be easily implemented in a short computational time.
Oliveira et al. [113] developed a mathematical model in which biofilm formation was coupled with heat transfer in a dual chamber MFC. Monod kinetics is used to predict substrate degradation fate and microbial growth. Acetate is the substrate and microbial growth is considered the growth of a microbial consortium.
Jayasinghe et al. [114] proposed a genome-scale flux balance analysis model using a Nernst-Monod equation to connect biofilm formation in the anode. The biofilm consisted of G. sulfurreducens DL1 and acetate was used as the substrate.
Recio-Garrido et al. [115] developed a combined bioelectrochemical-electrical (CBE) MFC model considering two microbial populations, methanogenic archaea and exoelectrogenic bacteria. Acetate was the substrate used; degradation and microbial growth were modelled based on double and simple Monod kinetics. With this model, physical and electrical parameters can be estimated in real-time, thus enabling process optimization. Recio-Garrido et al. [116] proposed a CBE model based on acetate biodegradation using anaerobic sludge performing parameter estimation and sensitivity analysis.
Esfandyari et al. developed a mathematical model for batch mode [117] as well as continuous mode [118] in a dual-chamber MFC with a pure culture of Shewanella and lactate as the substrate. In the study where MFC operated in the batch mode, three different kinetics models, Monod kinetics, the Blackman model, and the Tessier model, were investigated to estimate the microorganism growth rate. In the model where the MFC operated in the continuous condition the Nerst–Monod equation was used to model substrate degradation and microbial growth kinetics.
Karamzadeh et al. [119] developed a mathematical model based on an anode with mixed bacteria. In this model, different concentrations of substrate, which is dairy wastewater, are predicted using the Nernst–Monod expression.
6. Models Used for Microbial Growth Kinetics
In Table 3, the most common empirical and unstructured microbial growth kinetics models used in MFCs are presented. In these models, microbial growth kinetics are based on the Monod kinetics model and Monod-type models which may also include parameter(s) related to inhibition or consider more than one substrate as the limiting factors.
Table 3.
Common microbial growth kinetics models used in MFC processes.
7. Proposed Concept
The typical microbial growth kinetics models assume the substrate as the limiting factor, the presence of an inhibitor is also assumed, however there is lack of insight information and the process is a black box. However, many interactions at gene and enzyme level take place leading to substrate biodegradation, and biomass and product formation. Therefore, gene regulation plays a key role in microbial growth kinetics models and is currently overlooked.
The proposed concept is based on that reported in Tsipa et al. [11], in which the dynamic modelling of the gene regulatory network of the main metabolic pathway of the TOL (pWW0) plasmid of P. putida mt-2 activated upon exposure to mixed pollutants was studied. The gene regulatory network model utilized consistent time-series data of transcriptional kinetics obtained through quantitative polymerase chain reaction (qPCR). Following this, the gene regulatory network model was connected to growth kinetics (GK), leading to prediction of substrate biodegradation kinetics and microbial growth. The Tsipa et al. [11] study also predicted optimal bioprocess design through model-based control at the gene level. The efficient predictive capability of the Tsipa et al. [11] model was proved through comparison with four typical Monod and Monod-type kinetics for a double substrate (Figure 1). The values of model parameters of the four models and the Tsipa et al. model are presented as Supplementary Material (Tables S1 and S2).
Figure 1.
Comparison of the predictions of Tsipa et al. [11] framework with four commonly used microbial growth kinetic models for double substrate biodegradation. In the first experiment, 0.7 mM of both m-xylene (A) and toluene (B) were used, while microbial growth (C) was monitored. In the second experiment, 0.4 mM of both m-xylene (D) and toluene (E) were used, while microbial growth (F) was monitored. In the third experiment, 0.7 mM of m-xylene (G) and 0.4 mM of toluene (H) were used, while microbial growth (I) was monitored. R2 was also determined for each model at each experimental condition, as shown in the Table. More details are discussed in Tsipa et al. [11].
Consequently, the concept of optimizing and controlling the biodegradation kinetics in MFC systems focuses on the main gene regulatory network, which is activated upon exposure to the substrate. Systematic time-series mRNA expression data regarding the key genes and/or promoters of the gene regulatory network can be obtained through qPCR. The transcriptional kinetics provide the dynamic nature of the mRNA expression of genes and/or promoters. Transcriptional kinetics can also deliver key information regarding the relationship between transcriptional factors and genes in the presence of substrates, enhancing our knowledge of the gene regulatory network [126,127]. mRNA expression is considered one of the essential steps ensuring protein expression. Hence, monitoring of the transcriptional kinetics is also informative for enzyme expression. A dynamic kinetic model based on the gene regulatory network is built based on Hill functions [128]; the latter describe the dependence of a gene on a transcriptional factor. Protein expression is also modelled, through mass balance equations. The tools to distinguish the most significant parameters and determine those parameters are sensitivity analysis and parameter estimation, respectively. There are several methods for performing sensitivity analysis (e.g., local, global) and parameter estimation. Models of biological systems are usually complex, with many parameters; combination of more than one identification methodology parameter can, therefore, result in more accurate predictions [129].
One of the enzymes of the metabolic pathway is considered the most important for substrate degradation and another for biomass growth and product formation [130]. Hence, the gene regulatory network model can be connected to the microbial growth kinetics model, where instead of having the substrate as the limiting factor, the limiting factor will be the gene responsible for the growth, biodegradation and product formation, respectively. Gene expression will be predicted through the gene regulatory network and, then, growth, substrate biodegradation (and product formation) kinetics will be effectively predicted through gene regulatory network kinetics prediction. Validation experiments, using different experimental data sets, should be performed in order to ensure the predictability of the framework and model credibility for model-based design and control of experiments, and for optimization of the biosystem [131,132].
Global sensitivity analysis leads to identification of the most significant parameters, and their changes affect the model variables. The parameters are mostly based on maximum expression, degradation and saturation of genes and enzymes. Through sensitivity analysis, the molecules which most affect the system are thus recognized, and can be controlled or engineered to enhance the bioprocess performance. In Tsipa et al. [11], the model validated led to the design of a fed-batch process based on the hybrid gene regulatory network model to increase the amount of pollutant which was degraded during the process. A key promoter was controlled. The model-based process was successfully validated experimentally, proving that a validated hybrid gene regulatory network-microbial growth kinetic model can result in optimization of the process (Figure 2).
Figure 2.
The framework reported in Tsipa et al. 2018 [11]. Transcriptional kinetics are the input for the gene regulatory network-microbial growth kinetic model to be built and validated. When the model is valid and has predictive capability, enzyme expression, substrate biodegradation and microbial growth can be predicted.
The Tsipa et al. [11] framework was also applied to an engineered genetic circuit in E. coli. The genetic circuit was designed and optimized to produce cellulose. The framework could predict cellulose production through the hybrid gene regulatory network-microbial growth kinetic model [130]. This framework can, therefore, be applied to different natural or engineered biosystems to predict bioprocess kinetics through the targeted gene regulatory network, thus enhancing bioprocess scaling-up.
Nonetheless, the application of such a framework is also challenging. The biodegradation kinetics and relevant metabolic pathways of recalcitrant pollutants have not been well understood, determined and assessed yet in MFCs and cannot easily be controlled due to the multiple microbes and gene regulatory networks involved. Only a few studies have focused on revealing the main metabolic pathway involved in biodegradation. Hence, in-depth fundamental research is essential for understanding and defining the biochemical reactions for pollutants degradation, biomass and product formation, and metabolic pathways related to a specific microbial strain and/or community in an MFC system. Basic research needs to start by revealing the biodegradation metabolic pathway and gene regulation of one substrate in one microorganism. Furthermore, it should be combined with the knowledge already acquired for the gene regulation of recalcitrant pollutants in MFC model microorganisms, such as Pseudomonas spp., as mentioned above. These fundamentals are necessary for optimization, control and scale up of this technology to render it an industrial process. Furthermore, as waste, wastewater and polluted soil is a matrix of pollutants, this can be the basis for combining more substrates which are degraded through other metabolic pathways, and more microorganisms.
8. MFC Control, Monitoring and Applications
In the last few years, technological advances in the fields of electronics and material science have reduced the energy needed to power electronic devices, like the power consumption of wireless sensor networks (WSNs). Low-power and ultra-low power electronic devices make it possible to design electronic systems characterized by ultra-low energy consumption and use power sources based on energy harvesting techniques that involve clean, renewable sources. An energy harvesting technology such as a microbial fuel cell can produce power suitable for the normal operation of a wireless sensor network [133]. Furthermore, MFCs can be used as a biosensor, a bioreactor and a bio-decontaminator. These features are all useful for the functioning of nodes in a wireless sensor network for environmental monitoring. Moreover, their use as a bioreactor can provide the energy supply of devices such as microcomputers and mobile phones [134]. The proper set-up for analyzing MFC performance and adapting an energy management system able to supply a WSN node includes stable and monitored boundary conditions and appropriate measurement systems. As a matter of fact, an adapted measuring instrument is necessary for performing correct surveys of the electrical characteristics of MFCs and building accurate mathematical models. In order to perform accurate measurement and characterize MFC cells from an electrical point of view, it is necessary to use dedicated and programmable instruments. Solutions with current commercial devices are expensive and also not especially suitable for the electrical characterization of MFCs. Preferably, customised electronic boards dedicated to MFC measurement and analysis should be created [135]. A survey is presented here on the possible choices for energy conversion and management, transceiver devices and transmission protocol needed to exploit MFC performances to power a WSN node. A monitoring system needs to include a power management system with a DC/DC converter. It is necessary to adapt the level of the energy collected from the MFC to the needs of the system. A transceiver module is required for transmission of data that can be collected from a low power sensor node or from the MFC itself [136]. Figure 3 shows a panoramic view of an environmental monitoring and depollution system based on MFCs.
Figure 3.
Environmental monitoring system based on a wireless sensor network (WSN) and MFC.
Table 4 reports a list of the characteristics for some commercial transceivers which constitute a WSN node in combination with a sensor. The active Tx current required in transmission, the current consumption in “sleep mode”, the supply range and the frequency used are reported. The transceiver systems by Texas Instruments are the CC1310 Wireless MCU containing an ARM Cortex-M3 (CM3) 32-bit central processing unit (CPU) and the CC2533, which combines the performance of an RF transceiver with a single-cycle compliant CPU. The CC2533 is an optimized system-on-chip (SoC) solution for IEEE 802.15.4 based remote-control systems such as ZigBee.
Table 4.
Comparison of low power transceivers suitable for WSN empowered by MFCs.
The energy produced by MFCs can be used to power a WSN node, allowing the realization of applications such as ambient monitoring and precision farming without environmental impact [133,137,138]. Every network node includes a transceiver for communication, and generally a microcontroller for local operation and signal processing. An MFC usually delivers current and voltage values that are lower than those needed for the operation of these devices. In order to reach adequate levels of current and voltage, an energy management system is required. Since MFCs produce a level of voltage insufficient to support what a WSN node requires, the energy needs to be stored during the standby/idle time of the system. The “energy storage” operation mode is needed until the energy stored reaches the amount required to support the proper operation of a WSN node, data elaboration and transmission. For these reasons, the design of power management systems includes a step-up direct current (DC)/DC converter to boost the voltage and the power production of MFCs.
In Table 5 the principal properties and voltage requirements for some commercial low-power converters, including efficiency and quiescent current delivered (IQ), are listed. The start-up voltage is the critical threshold needed to allow the functioning of the system. The LTC 3108 and LTC 3105 converters by linear technologies are presented as the Enocean ECT 310 Perpetuum. Moreover, the LTC 3105 has the feature of fractional open circuit voltage (FOCV). The S-882Z produced by Seiko, which has a start-up input voltage of 300 mV, is also shown. On the other hand, the BQ25504 by Texas instruments is a boost converter, which can be started with a VIN as low as 330 mV but once started, can continue to harvest energy down to VIN = 80 mV. It also has integrated programmable dynamic maximum power point tracking (MPPT). The MAX17222 has the highest efficiency of 0.95 but needs a start-up voltage of 400 mV.
Table 5.
Energy harvesting low power direct current DC/DC converter comparison.
The decrease of threshold input voltage to values lower than silicon diode threshold is obtained by the innovation such as new planar technology for transistor MOS manufacture. From conventional FinFET devices manufacturing to ultra-thin body and buried oxide fully depleted silicon on insulator (UTBB-FD-SOI). The last one technology uses an ultra-thin layer of insulator, named buried oxide (BOX), positioned on top of the base Silicon, and a very thin silicon film that implements the transistor channel. The film is so thin that is no need to dope the channel, and the transistor is Fully Depleted. This technology allows superior electrostatic control of the gate on the channel of the transistor, accomplished by efficient body biasing, which provides faster switching speeds.
Although there are different commercial systems available, The LTC 3108 is the DC/DC converter most utilised in recent papers [139,140,141] for the energy management systems powered by MFC. One of the reasons is the very low voltage start-up needed for the converter.
9. Conclusions
In this study, an advanced framework to predict microbial growth kinetics using gene regulation information is proposed. This study is also focused on: highlighting the MFC broad applicability, the most common microorganisms used in MFCs and the level of genomic insights of the microbes used. Furthermore, the most common mathematical modelling approaches, and microbial growth kinetics models used in MFCs are described to highlight the current gap in mathematical modelling of microbial growth kinetics modeling in MFCs.
Given the possibility of using MFCs with various fuels such as wastewater and soil, there are several possible areas of application. Among industrial applications, many options are available. In the agro-industrial sector, MFCs can be a valuable tool for remediating organic and inorganic pollutants. They are suitable for organic content degradation in wastewater, allowing a water reuse for irrigation purposes. As an example, coffee plantations and industries are one of the most interesting applications due to the high level of organic load in the wastewater which comes out from the industrial process. At the same time, an MFC can operate as a bioreactor providing energy for the operation of a monitoring network able to provide various information about the state of the system. Another emerging application of MFC technology is the recovery of soil and water from contamination. Indeed, MFCs can be used as bio-remediators to decrease organic and inorganic pollution of soil. They can be used in open terrain or as a closed reactor. The recovery from heavy metal contamination of soil is also a promising application for soil-based MFCs.
Comprehensive mathematical modelling, combining microbial growth kinetics and electrochemical reactions, can result in control, optimization and optimal design of the biosystem, thus leading to effective scaling-up. The empirical and unstructured Monod and Monod-type models are traditionally used to predict microbial growth and substrate biodegradation in MFC systems. These black box models lack fit and predictability. Moreover, the importance of the substrate in the system is underestimated. Insights into gene regulation combined with a microbial growth kinetic model may overcome this issue. Such a framework is proposed in this manuscript. Fundamental research to enhance the knowledge of microbial metabolism and gene regulation is imperative to achieve this.
Environmental monitoring with WSNs is one of the emerging applications for the energy recovered by MFCs; it provides environmental data gathering (such as temperature, wind force, weather, irrigation level, desertification) in harsh environments or in the absence of energy networks. Moreover, MFCs can be valuable systems for precision farming. Another significant commercial application can be their use as a bioreactor enabling the recharging of portable phones and laptops in the form of USB (5 V) recharger.
Supplementary Materials
Parameters of Tsipa et al. and the four Monod-type models used. The following are available online at https://www.mdpi.com/article/10.3390/pr9061038/s1, Table S1: Nomenclature and model parameter values of Tsipa et al. model, Table S2: Parameter values estimated for the double Monod, Mankad and Bungay, SKIP and the sum kinetics with competitive enzymatic interactions models.
Author Contributions
Individual contributions: conceptualization A.T. and A.P. Writing A.T., C.K.V. and A.P. Review and editing P.G. and V.F. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding. The APC was funded by CA19123 COST ACTION PHOENIX.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Acknowledgments
We acknowledge the COST Action Horizon program and the COST Action PHOENIX: Protection, resilience, rehabilitation of damaged environment (CA19123).
Conflicts of Interest
The authors declare no conflict of interest.
References
- Hassan, H.; Dai, S.; Jin, B. Bioelectrochemical Reaction Kinetics, Mechanisms, and Pathways of Chlorophenol Degradation in MFC Using Different Microbial Consortia. ACS Sustain. Chem. Eng. 2019, 7, 17263–17272. [Google Scholar] [CrossRef] [Scilit]
- Walter, X.A.; Greenman, J.; Ieropoulos, I.A. Microbial fuel cells directly powering a microcomputer. J. Power Sources 2020, 446, 227328. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jadhav, D.A.; Carmona-Martínez, A.A.; Chendake, A.D.; Pandit, S.; Pant, D. Modeling and optimization strategies towards performance enhancement of microbial fuel cells. Bioresour. Technol. 2021, 320, 124256. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bailey, J.E. Biochemical Engineering Fundamentals; McGAraw-Hill: New York, NY, USA, 1986. [Google Scholar]
- Monod, J. The growth of bacterial cultures. Annu. Rev. Microbiol. 1949, 3, 371–394. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Zheng, P.; Zhang, M.; Chen, H.; Chen, T.; Xie, Z.; Cai, J.; Abbas, G. Kinetics of substrate degradation and electricity generation in anodic denitrification microbial fuel cell (AD-MFC). Bioresour. Technol. 2013, 149, 44–50. [Google Scholar] [CrossRef] [Scilit]
- Gadkari, S.; Shemfe, M.; Sadhukhan, J. Microbial fuel cells: A fast converging dynamic model for assessing system performance based on bioanode kinetics. Int. J. Hydrogen Energy 2019, 44, 15377–15386. [Google Scholar] [CrossRef] [Scilit]
- Miroliaei, M.R.; Samimi, A.; Mohebbi-Kalhori, D.; Khorram, M. Kinetics investigation of diversity cultures of E. coli and Shewanella sp., and their combined effect with mediator on MFC performance. J. Ind. Eng. Chem. 2015, 25, 42–50. [Google Scholar] [CrossRef] [Scilit]
- King, R. A structured mathematical model for a class of organisms: I. Development of a model for Streptomyces tendae and application of model-based control. J. Biotechnol. 1997, 52, 219–234. [Google Scholar] [CrossRef] [Scilit]
- Kovarova-Kovar, K.; Egli, T. Growth Kinetics of Suspended Microbial Cells: From Single- Substrate-Controlled Growth to Mixed-Substrate Kinetics. Microbiol. Mol. Biol. Rev. 1998, 62, 646–666. [Google Scholar] [CrossRef] [Scilit]
- Tsipa, A.; Koutinas, M.; Usaku, C.; Mantalaris, A. Optimal bioprocess design through a gene regulatory network—Growth kinetic hybrid model: Towards replacing Monod kinetics. Metab. Eng. 2018, 48, 129–137. [Google Scholar] [CrossRef] [Scilit]
- Gadkari, S.; Gu, S.; Sadhukhan, J. Towards automated design of bioelectrochemical systems: A comprehensive review of mathematical models. Chem. Eng. J. 2018, 343, 303–316. [Google Scholar] [CrossRef] [Scilit]
- Fang, C.; Achal, V. The potential of microbial fuel cells for remediation of heavy metals from soil and water—Review of application. Microorganisms 2019, 7, 697. [Google Scholar] [CrossRef] [Scilit]
- Yang, K.; Ji, M.; Liang, B.; Zhao, Y.; Zhai, S.; Ma, Z.; Yang, Z. Bioelectrochemical degradation of monoaromatic compounds: Current advances and challenges. J. Hazard. Mater. 2020, 398, 122892. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kronenberg, M.; Trably, E.; Bernet, N.; Patureau, D. Biodegradation of polycyclic aromatic hydrocarbons: Using microbial bioelectrochemical systems to overcome an impasse. Environ. Pollut. 2017, 231, 509–523. [Google Scholar] [CrossRef] [Scilit]
- Mandal, S.K.; Das, N. Application of microbial fuel cells for bioremediation of environmental pollutants: An overview. J. Microbiol. Biotechnol. Food Sci. 2018, 7, 437–444. [Google Scholar] [CrossRef] [Scilit]
- Wuana, R.A.; Okieimen, F.E. Heavy Metals in Contaminated Soils: A Review of Sources, Chemistry, Risks and Best Available Strategies for Remediation. ISRN Ecol. 2011, 2011, 1–20. [Google Scholar] [CrossRef] [Scilit]
- Saba, B.; Khan, M.; Christy, A.D.; Kjellerup, B.V. Microbial phyto-power systems—A sustainable integration of phytoremediation and microbial fuel cells. Bioelectrochemistry 2019, 127, 1–11. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Cao, X.; Wang, H.; Long, X.; Li, X. Simultaneous enhancement of heavy metal removal and electricity generation in soil microbial fuel cell. Ecotoxicol. Environ. Saf. 2020, 192, 110314. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, M.; Zhou, S.; Xu, Y.; Liu, Z.; Ma, F.; Zhi, L.; Zhou, X. Simultaneous Cr (VI) reduction and bioelectricity generation in a dual chamber microbial fuel cell. Chem. Eng. J. 2018, 334, 1621–1629. [Google Scholar] [CrossRef] [Scilit]
- Zhang, T.; Hu, L.; Zhang, M.; Jiang, M.; Fiedler, H. Cr (VI) removal from soils and groundwater using an integrated adsorption and microbial fuel cell (A-MFC) technology. Environ. Pollut. 2019, 252, 1399–1405. [Google Scholar] [CrossRef] [Scilit]
- Ali, J.; Wang, L.; Waseem, H.; Djellabi, R.; Oladoja, N.A.; Pan, G. FeS@rGO nanocomposites as electrocatalysts for enhanced chromium removal and clean energy generation by microbial fuel cell. Chem. Eng. J. 2020, 384, 123335. [Google Scholar] [CrossRef] [Scilit]
- Habibul, N.; Hu, Y.; Sheng, G. Microbial fuel cell driving electrokinetic remediation of toxic metal contaminated soils. J. Hazard. Mater. 2016, 318, 9–14. [Google Scholar] [CrossRef] [Scilit]
- Song, T.S.; Zhang, J.; Hou, S.; Wang, H.; Zhang, D.; Li, S.; Xie, J. In situ electrokinetic remediation of toxic metal-contaminated soil driven by solid phase microbial fuel cells with a wheat straw addition. J. Chem. Technol. Biotechnol. 2018, 93, 2860–2867. [Google Scholar] [CrossRef] [Scilit]
- Abourached, C.; Catal, T.; Liu, H. Efficacy of single-chamber microbial fuel cells for removal of cadmium and zinc with simultaneous electricity production. Water Res. 2014, 51, 228–233. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Colantonio, N.; Kim, Y. Cadmium (II) removal mechanisms in microbial electrolysis cells. J. Hazard. Mater. 2016, 311, 134–141. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Choi, C.; Hu, N.; Lim, B. Bioresource Technology Cadmium recovery by coupling double microbial fuel cells. Bioresour. Technol. 2014, 170, 361–369. [Google Scholar] [CrossRef] [Scilit]
- Li, M.; Zhou, S.; Xu, Y. Performance of Pb (II) reduction on di ff erent cathodes of microbial electrolysis cell driven by Cr (VI)-reduced microbial fuel cell. J. Power Sources 2019, 418, 1–10. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; He, Q.; Xia, L.; Li, Y.; Song, S. Algae cathode microbial fuel cells for cadmium removal with simultaneous electricity production using nickel foam/graphene electrode. Biochem. Eng. J. 2018, 138, 179–187. [Google Scholar] [CrossRef] [Scilit]
- Ancona, V.; Caracciolo, A.B.; Borello, D.; Ferrara, V.; Grenni, P.; Pietrelli, A. Microbial fuel cell: An energy harvesting technique for environmental remediation. Int. J. Environ. Impacts 2020, 3, 168–179. [Google Scholar] [CrossRef] [Scilit]
- Borello, D.; Gagliardi, G.; Aimola, G.; Ancona, V.; Grenni, P.; Bagnuolo, G.; Garbini, G.L.; Rolando, L.; Barra Caracciolo, A. Use of microbial fuel cells for soil remediation: A preliminary study on DDE. Int. J. Hydrogen Energy 2021, 46, 10131–10142. [Google Scholar] [CrossRef] [Scilit]
- Izallalen, M.; Mahadevan, R.; Burgard, A.; Postier, B.; Didonato, R.; Sun, J.; Schilling, C.H.; Lovley, D.R. Geobacter sulfurreducens strain engineered for increased rates of respiration. Metab. Eng. 2008, 10, 267–275. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, S.; Zhang, H.; Li, Y.; Zhang, H.; Wang, O.; Zhang, J.; Liu, F. Co-occurrence of Methanosarcina mazei and Geobacteraceae in an iron (III)-reducing enrichment culture. Front. Microbiol. 2015, 6, 942. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Logan, B.E. Extracting Hydrogen and Electricity from Renewable Resources. Environ. Sci. Technol. 2004, 38, 160A–167A. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Orellana, R.; Leavitt, J.J.; Comolli, L.R.; Csencsits, R.; Janot, N.; Flanagan, K.A.; Gray, A.S.; Leang, C.; Izallalen, M.; Mester, T.; et al. U(VI) reduction by diverse outer surface c-type cytochromes of Geobacter sulfurreducens. Appl. Environ. Microbiol. 2013, 79, 6369–6374. [Google Scholar] [CrossRef] [Scilit]
- Inoue, K.; Leang, C.; Franks, A.E.; Woodard, T.L.; Nevin, K.P.; Lovley, D.R. Specific localization of the c-type cytochrome OmcZ at the anode surface in current-producing biofilms of Geobacter sulfurreducens. Environ. Microbiol. Rep. 2011, 3, 211–217. [Google Scholar] [CrossRef] [Scilit]
- Malvankar, N.S.; Lovley, D.R. Microbial nanowires: A new paradigm for biological electron transfer and bioelectronics. ChemSusChem 2012, 5, 1039–1046. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nevin, K.P.; Richter, H.; Covalla, S.F.; Johnson, J.P.; Woodard, T.L.; Orloff, A.L.; Jia, H.; Zhang, M.; Lovley, D.R. Power output and columbic efficiencies from biofilms of Geobacter sulfurreducens comparable to mixed community microbial fuel cells. Environ. Microbiol. 2008, 10, 2505–2514. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ishii, S.; Watanabe, K.; Yabuki, S.; Logan, B.E.; Sekiguchi, Y. Comparison of electrode reduction activities of Geobacter sulfurreducens and an enriched consortium in an air-cathode microbial fuel cell. Appl. Environ. Microbiol. 2008, 74, 7348–7355. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Reguera, G.; Nevin, K.P.; Nicoll, J.S.; Covalla, S.F.; Woodard, T.L.; Lovley, D.R. Biofilm and nanowire production leads to increased current in Geobacter sulfurreducens fuel cells. Appl. Environ. Microbiol. 2006, 72, 7345–7348. [Google Scholar] [CrossRef] [Scilit]
- Reguera, G.; McCarthy, K.D.; Mehta, T.; Nicoll, J.S.; Tuominen, M.T.; Lovley, D.R. Extracellular electron transfer via microbial nanowires. Nature 2005, 435, 1098–1101. [Google Scholar] [CrossRef] [Scilit]
- Richter, H.; McCarthy, K.; Nevin, K.P.; Johnson, J.P.; Rotello, V.M.; Lovley, D.R. Electricity generation by Geobacter sulfurreducens attached to gold electrodes. Langmuir 2008, 24, 4376–4379. [Google Scholar] [CrossRef] [Scilit]
- Smith, J.A.; Lovley, D.R.; Tremblay, P.L. Outer cell surface components essential for Fe (III) oxide reduction by Geobacter metallireducens. Appl. Environ. Microbiol. 2013, 79, 901–907. [Google Scholar] [CrossRef] [Scilit]
- Min, B.; Cheng, S.; Logan, B.E. Electricity generation using membrane and salt bridge microbial fuel cells. Water Res. 2005, 39, 1675–1686. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sun, D.; Wang, A.; Cheng, S.; Yates, M.; Logan, B.E. Geobacter anodireducens sp. nov., an exoelectrogenic microbe in bioelectrochemical systems. Int. J. Syst. Evol. Microbiol. 2014, 64, 3485–3491. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Summers, Z.M.; Fogarty, H.E.; Leang, C.; Franks, A.E.; Malvankar, N.S.; Lovley, D.R. Direct exchange of electrons within aggregates of an evolved syntrophic coculture of anaerobic bacteria. Science 2010, 330, 1413–1415. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Smith, J.A.; Nevin, K.P.; Lovley, D.R. Syntrophic growth via quinone-mediated interspecies electron transfer. Front. Microbiol. 2015, 6, 121. [Google Scholar] [CrossRef] [Scilit]
- Shrestha, P.M.; Rotaru, A.E.; Aklujkar, M.; Liu, F.; Shrestha, M.; Summers, Z.M.; Malvankar, N.; Flores, D.C.; Lovley, D.R. Syntrophic growth with direct interspecies electron transfer as the primary mechanism for energy exchange. Environ. Microbiol. Rep. 2013, 5, 904–910. [Google Scholar] [CrossRef] [Scilit]
- Rotaru, A.E.; Shrestha, P.M.; Liu, F.; Shrestha, M.; Shrestha, D.; Embree, M.; Zengler, K.; Wardman, C.; Nevin, K.P.; Lovley, D.R. A new model for electron flow during anaerobic digestion: Direct interspecies electron transfer to Methanosaeta for the reduction of carbon dioxide to methane. Energy Environ. Sci. 2014, 7, 408–415. [Google Scholar] [CrossRef] [Scilit]
- Liu, F.; Rotaru, A.E.; Shrestha, P.M.; Malvankar, N.S.; Nevin, K.P.; Lovley, D.R. Promoting direct interspecies electron transfer with activated carbon. Energy Environ. Sci. 2012, 5, 8982–8989. [Google Scholar] [CrossRef] [Scilit]
- Kotloski, N.J.; Gralnick, J.A. Flavin electron shuttles dominate extracellular electron transfer by Shewanella oneidensis. MBio 2013, 4, e00553-12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gorby, Y.A.; Yanina, S.; McLean, J.S.; Rosso, K.M.; Moyles, D.; Dohnalkova, A.; Beveridge, T.J.; Chang, I.S.; Kim, B.H.; Kim, K.S.; et al. Electrically conductive bacterial nanowires produced by Shewanella oneidensis strain MR-1 and other exoelectrogens. Proc. Natl. Acad. Sci. USA 2006, 103, 11358–11363. [Google Scholar] [CrossRef] [Scilit]
- Baron, D.; LaBelle, E.; Coursolle, D.; Gralnick, J.A.; Bond, D.R. Electrochemical measurement of electron transfer kinetics by Shewanella oneidensis MR-1. J. Biol. Chem. 2009, 284, 28865–28873. [Google Scholar] [CrossRef] [Scilit]
- Von Canstein, H.; Ogawa, J.; Shimizu, S.; Lloyd, J.R. Secretion of flavins by Shewanella species and their role in extracellular electron transfer. Appl. Environ. Microbiol. 2008, 74, 615–623. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ringeisen, B.R.; Henderson, E.; Wu, P.K.; Pietron, J.; Ray, R.; Little, B.; Biffinger, J.C.; Jones-Meehan, J.M. High power density from a miniature microbial fuel cell using Shewanella oneidensis DSP10. Environ. Sci. Technol. 2006, 40, 2629–2634. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jain, A.; Zhang, X.; Pastorella, G.; Connolly, J.O.; Barry, N.; Woolley, R.; Krishnamurthy, S.; Marsili, E. Electron transfer mechanism in Shewanella loihica PV-4 biofilms formed at graphite electrode. Bioelectrochemistry 2012, 87, 28–32. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marsili, E.; Baron, D.B.; Shikhare, I.D.; Coursolle, D.; Gralnick, J.A.; Bond, D.R. Shewanella secretes flavins that mediate extracellular electron transfer. Proc. Natl. Acad. Sci. USA 2008, 105, 3968–3973. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, W.; Yang, F.; Liu, X.; Bai, L. Influence of substrate on electricity generation of Shewanella loihica PV-4 in microbial fuel cells. Microb. Cell Fact. 2014, 13, 1–6. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pandit, S.; Khilari, S.; Roy, S.; Pradhan, D.; Das, D. Improvement of power generation using Shewanella putrefaciens mediated bioanode in a single chambered microbial fuel cell: Effect of different anodic operating conditions. Bioresour. Technol. 2014, 166, 451–457. [Google Scholar] [CrossRef] [Scilit]
- Pham, C.A.; Jung, S.J.; Phung, N.T.; Lee, J.; Chang, I.S.; Kim, B.H.; Yi, H.; Chun, J. A novel electrochemically active and Fe (III)-reducing bacterium phylogenetically related to Aeromonas hydrophila, isolated from a microbial fuel cell. FEMS Microbiol. Lett. 2003, 223, 129–134. [Google Scholar] [CrossRef] [Scilit]
- Dietrich, L.E.P.; Price-Whelan, A.; Petersen, A.; Whiteley, M.; Newman, D.K. The phenazine pyocyanin is a terminal signalling factor in the quorum sensing network of Pseudomonas aeruginosa. Mol. Microbiol. 2006, 61, 1308–1321. [Google Scholar] [CrossRef] [Scilit]
- Stoodley, P.; Sauer, K.; Davies, D.G.; Costerton, J.W. Biofilms as complex differentiated communities. Annu. Rev. Microbiol. 2002, 56, 187–209. [Google Scholar] [CrossRef] [Scilit]
- Rabaey, K.; Boon, N.; Höfte, M.; Verstraete, W. Microbial phenazine production enhances electron transfer in biofuel cells. Environ. Sci. Technol. 2005, 39, 3401–3408. [Google Scholar] [CrossRef] [Scilit]
- Fazli, M.; Almblad, H.; Rybtke, M.L.; Givskov, M.; Eberl, L.; Tolker-Nielsen, T. Regulation of biofilm formation in Pseudomonas and Burkholderia species. Environ. Microbiol. 2014, 16, 1961–1981. [Google Scholar] [CrossRef] [Scilit]
- Park, H.S.; Kim, B.H.; Kim, H.S.; Kim, H.J.; Kim, G.T.; Kim, M.; Chang, I.S.; Park, Y.K.; Chang, H.I. A novel electrochemically active and Fe (III)-reducing bacterium phylogenetically related to Clostridium butyricum isolated from a microbial fuel cell. Anaerobe 2001, 7, 297–306. [Google Scholar] [CrossRef] [Scilit]
- Singh, L.; Wahid, Z. Enhancement of hydrogen production from palm oil mill effluent via cell immobilisation technique. Int. J. Energy Res. 2014, 39, 215–222. [Google Scholar] [CrossRef] [Scilit]
- Wang, H.; Lu, L.; Cui, F.; Liu, D.; Zhao, Z.; Xu, Y. Simultaneous bioelectrochemical degradation of algae sludge and energy recovery in microbial fuel cells. RSC Adv. 2012, 7228–7234. [Google Scholar] [CrossRef] [Scilit]
- Cui, Y.; Rashid, N.; Hu, N.; Saif, M.; Rehman, U.; Han, J. Electricity generation and microalgae cultivation in microbial fuel cell using microalgae-enriched anode and bio-cathode. Energy Convers. Manag. 2014, 79, 674–680. [Google Scholar] [CrossRef] [Scilit]
- Kim, G.T.; Hyun, M.S.; Chang, I.S.; Kim, H.J.; Park, H.S.; Kim, B.H.; Kim, S.D.; Wimpenny, J.W.T.; Weightman, A.J. Dissimilatory Fe (III) reduction by an electrochemically active lactic acid bacterium phylogenetically related to Enterococcus gallinarum isolated from submerged soil. J. Appl. Microbiol. 2005, 99, 978–987. [Google Scholar] [CrossRef] [Scilit]
- Keogh, D.; Lam, L.N.; Doyle, L.E.; Matysik, A.; Pavagadhi, S.; Umashankar, S.; Low, P.M.; Dale, J.L.; Song, Y.; Ng, S.P.; et al. Extracellular Electron Transfer Powers Enterococcus faecalis Biofilm Metabolism. MBio 2018, 9, e00626-17. [Google Scholar] [CrossRef] [Scilit]
- El-Naggar, M.Y.; Wanger, G.; Leung, K.M.; Yuzvinsky, T.D.; Southam, G.; Yang, J.; Lau, W.M.; Nealson, K.H.; Gorby, Y.A. Electrical transport along bacterial nanowires from Shewanella oneidensis MR-1. Proc. Natl. Acad. Sci. USA 2010, 107, 18127–18131. [Google Scholar] [CrossRef] [Scilit]
- Zuo, Y.; Xing, D.; Regan, J.M.; Logan, B.E. Isolation of the exoelectrogenic bacterium Ochrobactrum anthropi YZ-1 by using a U-tube microbial fuel cell. Appl. Environ. Microbiol. 2008, 74, 3130–3137. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Parameswaran, P.; Bry, T.; Popat, S.C.; Lusk, B.G.; Rittmann, B.E.; Torres, C.I. Kinetic, electrochemical, and microscopic characterization of the thermophilic, anode-respiring bacterium Thermincola ferriacetica. Environ. Sci. Technol. 2013, 47, 4934–4940. [Google Scholar] [CrossRef] [Scilit]
- Wrighton, K.C.; Thrash, J.C.; Melnyk, R.A.; Bigi, J.P.; Byrne-Bailey, K.G.; Remis, J.P.; Schichnes, D.; Auer, M.; Chang, C.J.; Coates, J.D. Evidence for direct electron transfer by a gram-positive bacterium isolated from a microbial fuel cell. Appl. Environ. Microbiol. 2011, 77, 7633–7639. [Google Scholar] [CrossRef] [Scilit]
- Bond, D.R.; Lovley, D.R. Evidence for involvement of an electron shuttle in electricity generation by Geothrix fermentans. Appl. Environ. Microbiol. 2005, 71, 2186–2189. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mehta-Kolte, M.G.; Bond, D.R. Geothrix fermentans secretes two different redox-active compounds to utilize electron acceptors across a wide range of redox potentials. Appl. Environ. Microbiol. 2012, 78, 6987–6995. [Google Scholar] [CrossRef] [Scilit]
- Keller, K.L.; Rapp-Giles, B.J.; Semkiw, E.S.; Porat, I.; Brown, S.D.; Wall, J.D. New model for electron flow for sulfate reduction in Desulfovibrio alaskensis G20. Appl. Environ. Microbiol. 2014, 80, 855–868. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kang, C.S.; Eaktasang, N.; Kwon, D.Y.; Kim, H.S. Enhanced current production by Desulfovibrio desulfuricans biofilm in a mediator-less microbial fuel cell. Bioresour. Technol. 2014, 165, 27–30. [Google Scholar] [CrossRef] [Scilit]
- Freguia, S.; Masuda, M.; Tsujimura, S.; Kano, K. Lactococcus lactis catalyses electricity generation at microbial fuel cell anodes via excretion of a soluble quinone. Bioelectrochemistry 2009, 76, 14–18. [Google Scholar] [CrossRef] [Scilit]
- Kumar, R.; Singh, L.; Wahid, Z.A.; Din, M.F. Exoelectrogens in microbial fuel cells toward bioelectricity generation: A review. Int. J. Energy Res. 2015, 39, 1048–1067. [Google Scholar] [CrossRef] [Scilit]
- Qiao, Y.; Li, C.M.; Bao, S.J.; Lu, Z.; Hong, Y. Direct electrochemistry and electrocatalytic mechanism of evolved Escherichia coli cells in microbial fuel cells. Chem. Commun. 2008, 1290–1292. [Google Scholar] [CrossRef] [Scilit]
- Fuller, S.J.; McMillan, D.G.G.; Renz, M.B.; Schmidt, M.; Burke, I.T.; Stewart, D.I. Extracellular electron transport-mediated Fe (III) reduction by a community of alkaliphilic bacteria that use flavins as electron shuttles. Appl. Environ. Microbiol. 2014, 80, 128–137. [Google Scholar] [CrossRef] [Scilit]
- Lifang, D.; FrangBai, L.; Shungui, Z.; Yin, H.D.; Jinren, N.I. A study of electron-shuttle mechanism in Klebsiella pneumoniae based microbial fuel cells. Environ. Sci. Technol. 2010, 55, 99–104. [Google Scholar]
- Xing, D.; Zuo, Y.; Cheng, S.; Regan, J.M.; Logan, B.E. Electricity generation by Rhodopseudomonas palustris DX-1. Environ. Sci. Technol. 2008, 42, 4146–4151. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Inglesby, A.E.; Beatty, D.A.; Fisher, A.C. Rhodopseudomonas palustris purple bacteria fed Arthrospira maxima cyanobacteria: Demonstration of application in microbial fuel cells. RSC Adv. 2012, 2, 4829–4838. [Google Scholar] [CrossRef] [Scilit]
- Raghavulu, S.V.; Goud, R.K.; Sarma, P.N.; Mohan, S.V. Saccharomyces cerevisiae as anodic biocatalyst for power generation in biofuel cell: Influence of redox condition and substrate load. Bioresour. Technol. 2011, 102, 2751–2757. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Prasad, D.; Arun, S.; Murugesan, M.; Padmanaban, S.; Satyanarayanan, R.S.; Berchmans, S.; Yegnaraman, V. Direct electron transfer with yeast cells and construction of a mediatorless microbial fuel cell. Biosens. Bioelectron. 2007, 22, 2604–2610. [Google Scholar] [CrossRef] [Scilit]
- Hubenova, Y.; Mitov, M. Potential application of Candida melibiosica in biofuel cells. Bioelectrochemistry 2010, 78, 57–61. [Google Scholar] [CrossRef] [Scilit]
- Nandy, A.; Kumar, V.; Kundu, P.P. Utilization of proteinaceous materials for power generation in a mediatorless microbial fuel cell by a new electrogenic bacteria Lysinibacillus sphaericus VA5. Enzym. Microb. Technol. 2013, 53, 339–344. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xu, S.; Liu, H. New exoelectrogen Citrobacter sp. SX-1 isolated from a microbial fuel cell. J. Appl. Microbiol. 2011, 111, 1108–1115. [Google Scholar] [CrossRef] [Scilit]
- Kimura, Z.I.; Chung, K.M.; Itoh, H.; Hiraishi, A.; Okabe, S. Raoultella electrica sp. nov., isolated from anodic biofilms of a glucose-fed microbial fuel cell. Int. J. Syst. Evol. Microbiol. 2014, 64, 1384–1388. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, X.; Zhong, G.Z.; Qiao, Y.; Huang, J.; Hu, W.H.; Wang, X.G.; Li, C.M. A high performance xylose microbial fuel cell enabled by Ochrobactrum sp. 575 cells. RSC Adv. 2014, 4, 39839–39843. [Google Scholar] [CrossRef] [Scilit]
- Takeuchi, Y.; Khawdas, W.; Aso, Y.; Ohara, H. Microbial fuel cells using Cellulomonas spp. with cellulose as fuel. J. Biosci. Bioeng. 2017, 123, 358–363. [Google Scholar] [CrossRef] [Scilit]
- Khawdas, W.; Watanabe, K.; Karatani, H.; Aso, Y.; Tanaka, T.; Ohara, H. Direct electron transfer of Cellulomonas fimi and microbial fuel cells fueled by cellulose. J. Biosci. Bioeng. 2019, 128, 593–598. [Google Scholar] [CrossRef] [Scilit]
- Aslan, S.; Conghaile, P.Ó.; Leech, D.; Gorton, L.; Timur, S.; Anik, U. Development of an Osmium Redox Polymer Mediated Bioanode and Examination of its Performance in Gluconobacter oxydans Based Microbial Fuel Cell. Electroanalysis 2017, 29, 1651–1657. [Google Scholar] [CrossRef] [Scilit]
- Aslan, S.; Conghaile, P.Ó.; Leech, D.; Gorton, L.; Timur, S.; Anik, U. Development of a Bioanode for Microbial Fuel Cells Based on the Combination of a MWCNT-Au-Pt Hybrid Nanomaterial, an Osmium Redox Polymer and Gluconobacter oxydans DSM 2343 Cells. ChemistrySelect 2017, 2, 12034–12040. [Google Scholar] [CrossRef] [Scilit]
- Adachi, T.; Kitazumi, Y.; Shirai, O.; Kano, K. Direct electron transfer-type bioelectrocatalysis by membrane-bound aldehyde dehydrogenase from Gluconobacter oxydans and cyanide effects on its bioelectrocatalytic properties. Electrochem. Commun. 2021, 123, 106911. [Google Scholar] [CrossRef] [Scilit]
- Liu, X.; Ali, A.; Liu, C.; Liu, Y.; Zhang, P. The first in-depth exploration of the genome of the engineered bacterium, Gluconobacter thailandicus. Biotechnol. Appl. Biochem. 2021, 1–9. [Google Scholar] [CrossRef] [Scilit]
- Park, D.L.M.; Guettler, M.V.; Jain, M.K.; Zeikus, J.G. Microbial utilization of electrically reduced neutral red as the sole electron donor for growth and metabolite production. Appl. Environ. Microbiol. 1999, 65, 2912–2917. [Google Scholar] [CrossRef] [Scilit]
- Choudhury, P.; Uday, U.S.P.; Mahata, N.; Nath Tiwari, O.; Narayan Ray, R.; Kanti Bandyopadhyay, T.; Bhunia, B. Performance improvement of microbial fuel cells for waste water treatment along with value addition: A review on past achievements and recent perspectives. Renew. Sustain. Energy Rev. 2017, 79, 372–389. [Google Scholar] [CrossRef] [Scilit]
- Kouzuma, A.; Kasai, T.; Hirose, A.; Watanabe, K. Catabolic and regulatory systems in shewanella oneidensis MR-1 involved in electricity generation in microbial fuel cells. Front. Microbiol. 2015, 6, 609. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aklujkar, M.; Krushkal, J.; Dibartolo, G.; Lapidus, A.; Land, M.L.; Lovley, D.R. The genome sequence of Geobacter metallireducens: Features of metabolism, physiology and regulation common and dissimilar to Geobacter sulfurreducens. BMC Microbiol. 2009, 9, 1–22. [Google Scholar] [CrossRef] [Scilit]
- Heidelberg, J.F.; Paulsen, I.T.; Nelson, K.E.; Gaidos, E.J.; Nelson, W.C.; Read, T.D.; Eisen, J.A.; Seshadri, R.; Ward, N.; Methe, B.; et al. Genome sequence of the dissimilatory metal ion-reducing bacterium Shewanella oneidensis. Nat. Biotechnol. 2002, 20, 1118–1123. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Serres, M.H.; Riley, M. Genomic analysis of carbon source metabolism of Shewanella oneidensis MR-1: Predictions versus experiments. J. Bacteriol. 2006, 188, 4601–4609. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Deb, D.; Patel, R.; Balas, V.E. A Review of Control-Oriented Bioelectrochemical Mathematical Models of Microbial Fuel Cells. Processes 2020, 8, 583. [Google Scholar] [CrossRef] [Scilit]
- Jadhav, G.S.; Ghangrekar, M.M. Performance of microbial fuel cell subjected to variation in pH, temperature, external load and substrate concentration. Bioresour. Technol. 2009, 100, 717–723. [Google Scholar] [CrossRef] [Scilit]
- Merkey, B.V.; Chopp, D.L. The Performance of a Microbial Fuel Cell Depends Strongly on Anode Geometry: A Multidimensional Modeling Study. Bull. Math. Biol. 2012, 74, 834–857. [Google Scholar] [CrossRef] [Scilit]
- Ortiz-Martínez, V.M.; Salar-García, M.J.; de los Ríos, A.P.; Hernández-Fernández, F.J.; Egea, J.A.; Lozano, L.J. Developments in microbial fuel cell modeling. Chem. Eng. J. 2015, 271, 50–60. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Halme, A. Modelling of a Microbial Fuel Cell Process. Biotechnol. Lett. 1995, 17, 809–814. [Google Scholar] [CrossRef] [Scilit]
- Picioreanu, C.; van Loosdrecht, M.C.M.; Curtis, T.P.; Scott, K. Model based evaluation of the effect of pH and electrode geometry on microbial fuel cell performance. Bioelectrochemistry 2010, 78, 8–24. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zeng, Y.; Choo, Y.F.; Kim, B.H.; Wu, P. Modelling and simulation of two-chamber microbial fuel cell. J. Power Sources 2010, 195, 79–89. [Google Scholar] [CrossRef] [Scilit]
- Pinto, R.P.; Srinivasan, B.; Manuel, M.F.; Tartakovsky, B. A two-population bio-electrochemical model of a microbial fuel cell. Bioresour. Technol. 2010, 101, 5256–5265. [Google Scholar] [CrossRef] [Scilit]
- Oliveira, V.B.; Simões, M.; Melo, L.F.; Pinto, A.M.F.R. A 1D mathematical model for a microbial fuel cell. Energy 2013, 61, 463–471. [Google Scholar] [CrossRef] [Scilit]
- Jayasinghe, N.; Franks, A.; Nevin, K.P.; Mahadevan, R. Metabolic modeling of spatial heterogeneity of biofilms in microbial fuel cells reveals substrate limitations in electrical current generation. Biotechnol. J. 2014, 9, 1350–1361. [Google Scholar] [CrossRef] [Scilit]
- Recio-Garrido, D.; Perrier, M.; Tartakovsky, B. Parameter estimation of a microbial fuel cell process control-oriented model. In Proceedings of the 22nd Mediterranean Conference on Control and Automation, Palermo, Italy, 16–19 June 2014; pp. 918–923. [Google Scholar]
- Recio-Garrido, D.; Perrier, M.; Tartakovsky, B. Modeling, optimization and control of bioelectrochemical systems. Chem. Eng. J. 2016, 289, 180–190. [Google Scholar] [CrossRef] [Scilit]
- Esfandyari, M.; Fanaei, M.A.; Gheshlaghi, R.; Akhavan Mahdavi, M. Mathematical modeling of two-chamber batch microbial fuel cell with pure culture of Shewanella. Chem. Eng. Res. Des. 2017, 117, 34–42. [Google Scholar] [CrossRef] [Scilit]
- Esfandyari, M.; Fanaei, M.A.; Gheshlaghi, R.; Akhavan Mahdavi, M. Dynamic modeling of a continuous two-chamber microbial fuel cell with pure culture of Shewanella. Int. J. Hydrogen Energy 2017, 42, 21198–21202. [Google Scholar] [CrossRef] [Scilit]
- Karamzadeh, M.; Kadivarian, H.; Kadivarian, M.; Kazemi, A. Modeling the influence of substrate concentration, anode electrode surface area and external resistance in a start-up on the performance of microbial fuel cell. Bioresour. Technol. Rep. 2020, 12, 100559. [Google Scholar] [CrossRef] [Scilit]
- Pinto, R.P.; Srinivasan, B.; Escapa, A.; Tartakovsky, B. Multi-population model of a microbial electrolysis cell. Environ. Sci. Technol. 2011, 45, 5039–5046. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kato Marcus, A.; Torres, C.I.; Rittmann, B.E. Conduction-Based Modeling of the Biofilm Anode of a Microbial Fuel Cell. Biotechnol. Bioeng. 2007, 98, 1171–1182. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sirinutsomboon, B. Modeling of a membraneless single-chamber microbial fuel cell with molasses as an energy source. Int. J. Energy Environ. Eng. 2014, 5, 1–9. [Google Scholar] [CrossRef] [Scilit]
- Picioreanu, C.; Head, I.M.; Katuri, K.P.; van Loosdrecht, M.C.M.; Scott, K. A computational model for biofilm-based microbial fuel cells. Water Res. 2007, 41, 2921–2940. [Google Scholar] [CrossRef] [Scilit]
- Picioreanu, C.; Katuri, K.P.; Head, I.M.; Van Loosdrecht, M.C.M.; Scott, K. Mathematical model for microbial fuel cells with anodic biofilms and anaerobic digestion. Water Sci. Technol. 2008, 57, 965–971. [Google Scholar] [CrossRef] [Scilit]
- Jafary, T.; Ghoreyshi, A.A.; Najafpour, G.D.; Fatemi, S.; Rahimnejad, M. Investigation on performance of microbial fuel cells based on carbon sources and kinetic models. Int. J. Energy Res. 2013, 37, 1539–1549. [Google Scholar] [CrossRef] [Scilit]
- Tsipa, A.; Koutinas, M.; Pistikopoulos, E.N.; Mantalaris, A. Transcriptional kinetics of the cross-talk between the ortho-cleavage and TOL pathways of toluene biodegradation in Pseudomonas putida mt-2. J. Biotechnol. 2016, 228, 112–123. [Google Scholar] [CrossRef] [Scilit]
- Tsipa, A.; Koutinas, M.; Vernardis, S.; Mantalaris, A. The impact of succinate trace on pWW0 and ortho-cleavage pathway transcription in Pseudomonas putida mt-2 during toluene biodegradation. Bioresour. Technol. 2017, 234, 397–405. [Google Scholar] [CrossRef] [Scilit]
- Koutinas, M.; Kiparissides, A.; Silva-Rocha, R.; Lam, M.C.; Martins dos Santos, V.A.P.; de Lorenzo, V.; Pistikopoulos, E.N.; Mantalaris, A. Linking genes to microbial growth kinetics-An integrated biochemical systems engineering approach. Metab. Eng. 2011, 13, 401–413. [Google Scholar] [CrossRef] [Scilit]
- Tsipa, A.; Pitt, J.A.; Banga, J.R.; Mantalaris, A. A dual-parameter identification approach for data-based predictive modeling of hybrid gene regulatory network-growth kinetics in Pseudomonas putida mt-2. Bioprocess. Biosyst. Eng. 2020, 43, 1671–1688. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Buldum, G.; Tsipa, A.; Mantalaris, A. Linking Engineered Gene Circuit Kinetic Modeling to Cellulose Biosynthesis Prediction in Escherichia coli: Toward Bioprocessing of Microbial Cell Factories. Ind. Eng. Chem. Res. 2020, 59, 4659–4669. [Google Scholar] [CrossRef] [Scilit]
- Koutinas, M.; Kiparissides, A.; Pistikopoulos, E.N.; Mantalaris, A. Bioprocess systems engineering: Transferring traditional process engineering principles to industrial biotechnology. Comput. Struct. Biotechnol. J. 2012, 3, e201210022. [Google Scholar] [CrossRef] [Scilit]
- Kiparissides, A.; Koutinas, M.; Kontoravdi, C.; Mantalaris, A.; Pistikopoulos, E.N. “Closing the loop” in biological systems modeling-from the in silico to the in vitro. Automatica 2011, 47, 1147–1155. [Google Scholar] [CrossRef] [Scilit]
- Cooke, K.G.; Gay, M.O.; Radachowsky, S.E.; Guzman, J.J.; Chiu, M.A. BackyardNetTM: Distributed Sensor Network Powered by Terrestrial Microbial Fuel Cell. In Proceedings of the Unattended Ground, Sea, and Air Sensor Technologies and Applications XII. International Society for Optics and Photonics, Orlando, FL, USA, 5–8 April 2021. [Google Scholar]
- Prasad, J.; Tripathi, R.K. Scale-up and control the voltage of sediment microbial fuel cell for charging a cell phone. Biosens. Bioelectron. 2021, 172, 112767. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pietrelli, A.; Lovecchio, N.; Ferrara, V.; Allard, B. Custom measuring system tailored for MFCs. In Proceedings of the 2019 IEEE 8th International Workshop on Advances in Sensors and Interfaces (IWASI), Otranto, Italy, 13–14 June 2019; pp. 270–273. [Google Scholar]
- Logroño, W.; Guambo, A.; Pérez, M.; Kadier, A.; Recalde, C. A terrestrial single chamber microbial fuel cell-based biosensor for biochemical oxygen demand of synthetic ricewashed wastewater. Sensors 2016, 16, 101. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sartori, D.; Brunelli, D. A smart sensor for precision agriculture powered by micro-bial fuel cells. In Proceedings of the IEEE Sensors Applications Symposium (SAS), Catania, Italy, 20–22 April 2016; pp. 1–6. [Google Scholar]
- Rossi, M.; Tosato, P.; Gemma, L.; Torquati, L.; Catania, C.; Camalo, S.; Brunelli, D. Long range wireless sensing powered by plant-microbial fuel cell. In Proceedings of the Design, Automation & Test in Europe Conference & Exhibition (DATE), Lausanne, Switzerland, 27–31 March 2017; pp. 1651–1654. [Google Scholar]
- Song, Y.E.; Boghani, H.C.; Kim, H.S.; Kim, B.G.; Lee, T.; Jeon, B.H.; Premier, G.C.; Kim, J.R. Electricity production by the application of a low voltage DC-DC boost converter to a continuously operating flat-plate microbial fuel cell. Energies 2017, 10, 596. [Google Scholar] [CrossRef] [Scilit]
- Prasad, J.; Tripathi, R.K. A Dc-Dc Boost Converter for Sediment Microbial Fuel Cell Energy Harvesting. In Proceedings of the 2nd IEEE International Conference on Power Electronics, Intelligent Control and Energy Systems (ICPEICES), New Delhi, India, 22–24 October 2018; pp. 712–716. [Google Scholar]
- Kim, T.; Yeo, J.; Yang, Y.; Kang, S.; Paek, Y.; Kwon, J.K.; Jang, J.K. Boosting voltage without electrochemical degradation using energy-harvesting circuits and power management system-coupled multiple microbial fuel cells. J. Power Sources 2019, 410–411, 171–178. [Google Scholar] [CrossRef] [Scilit]
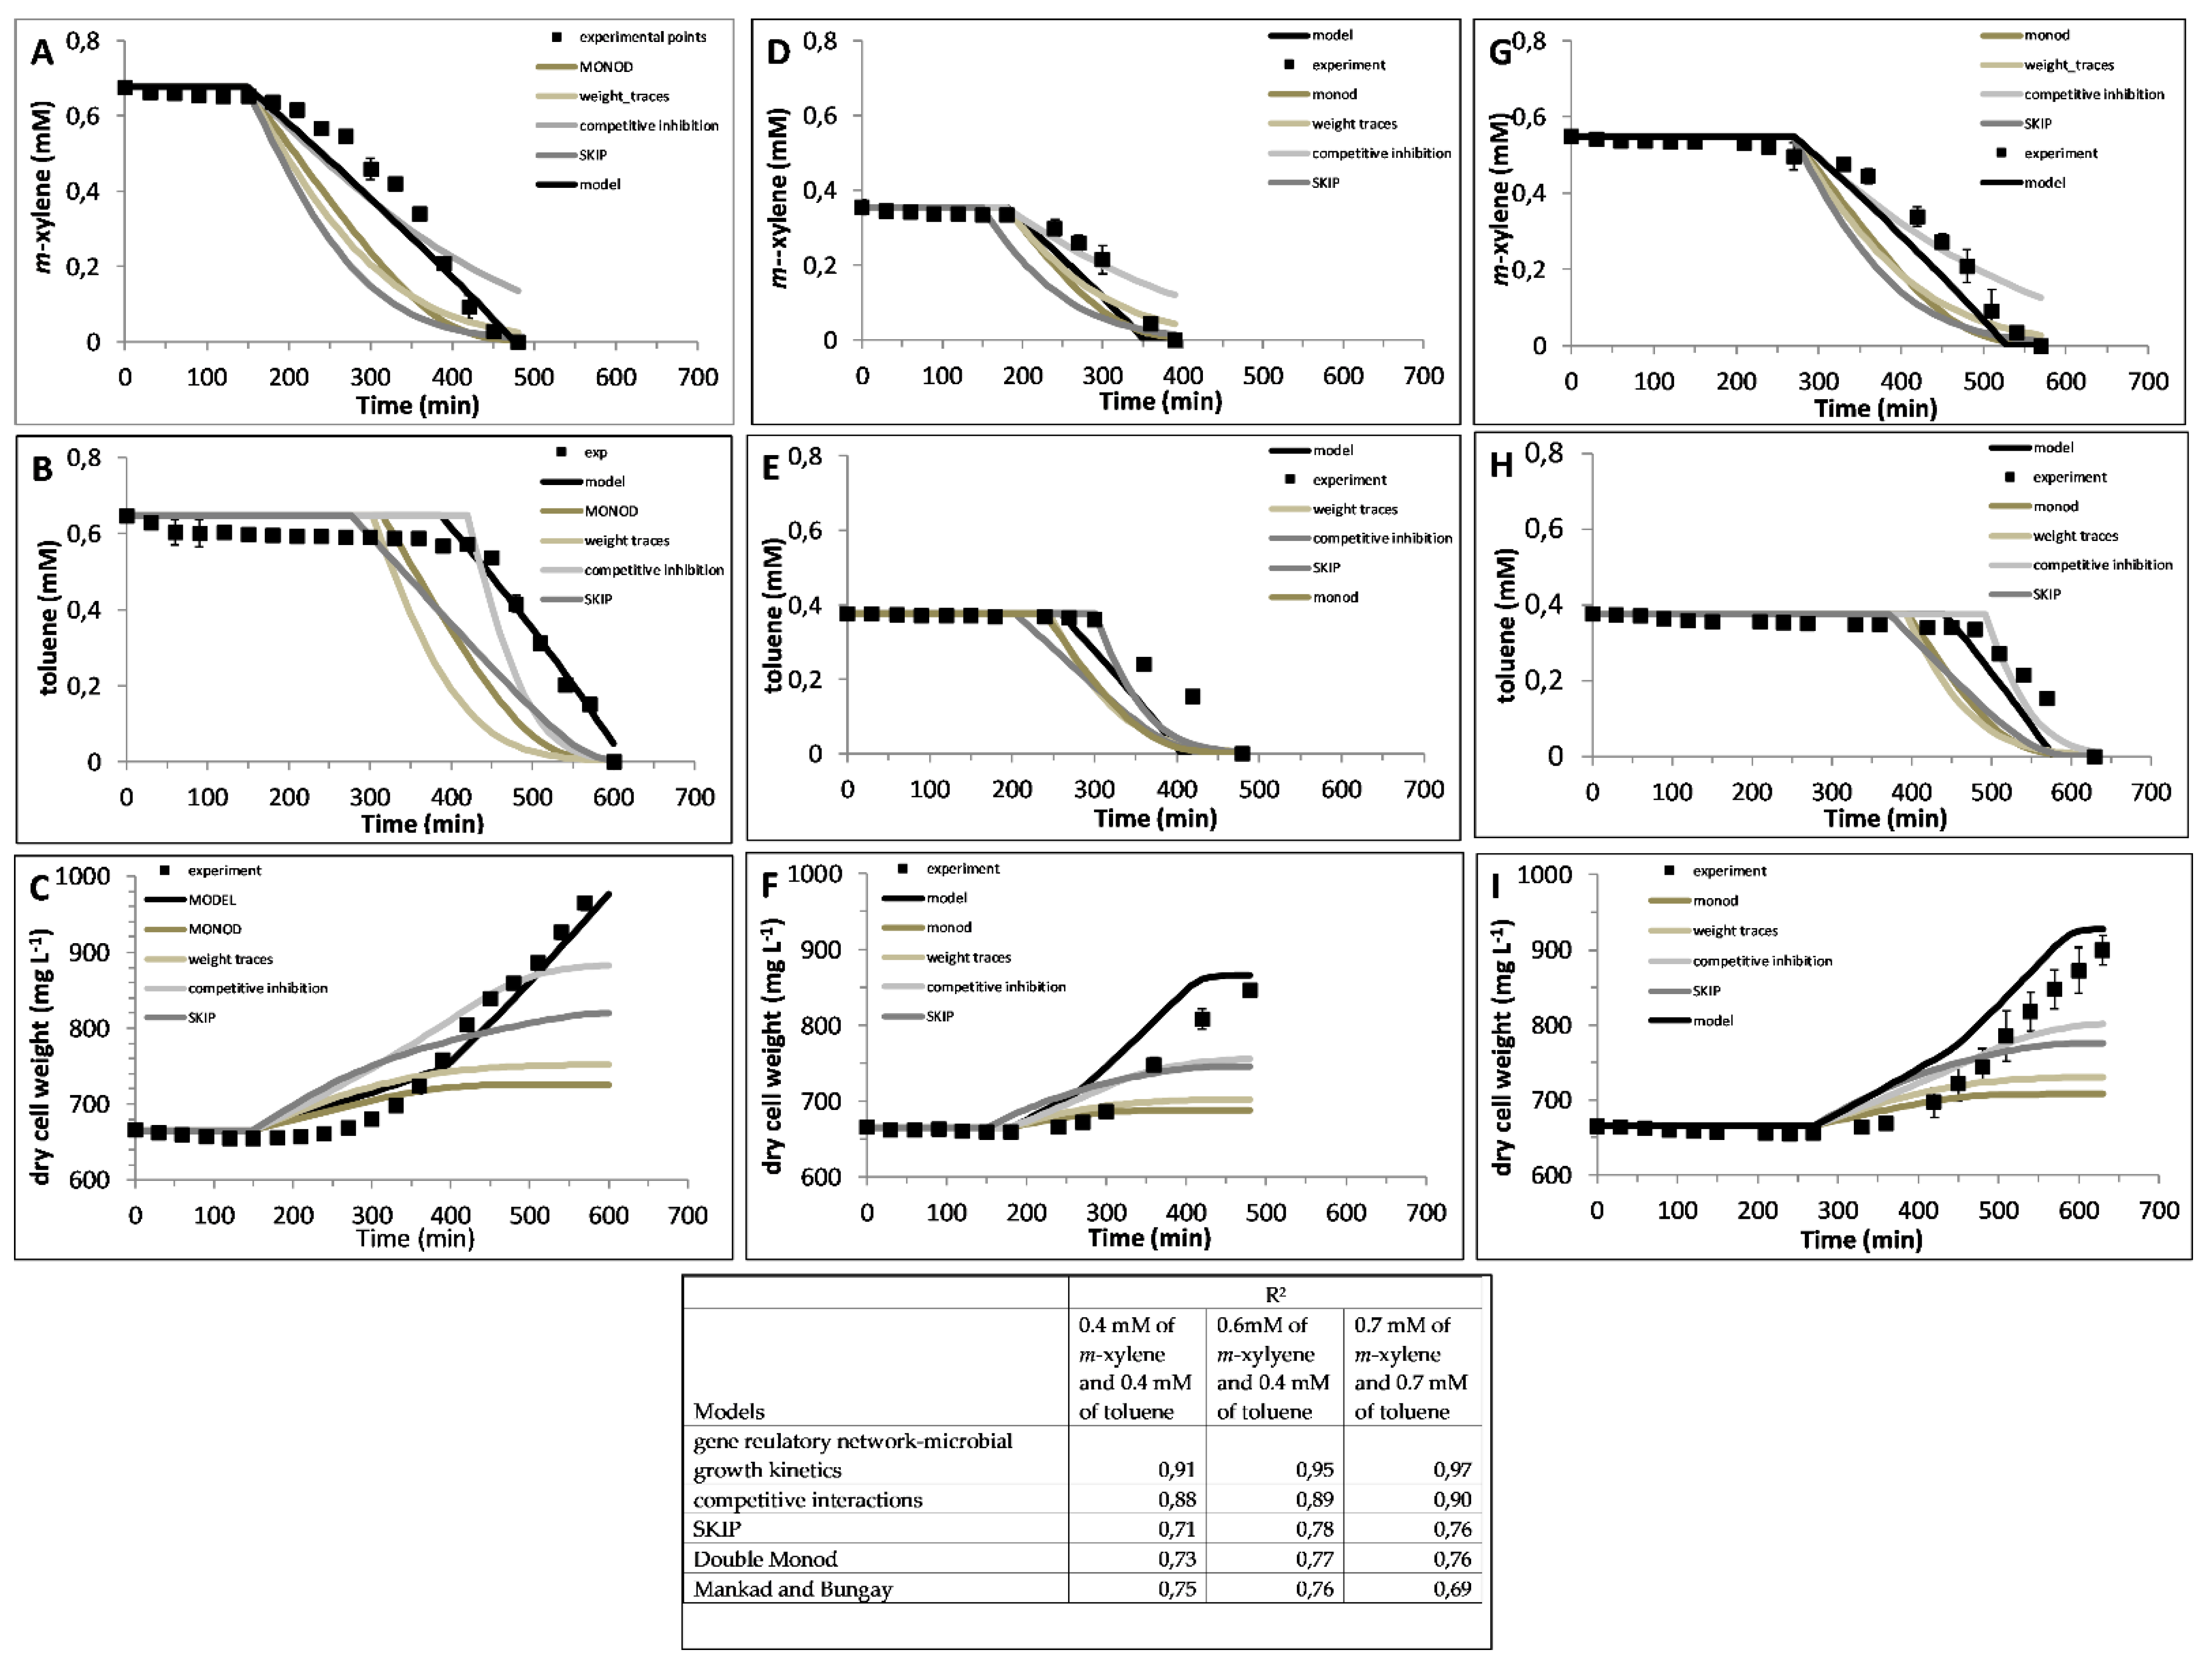
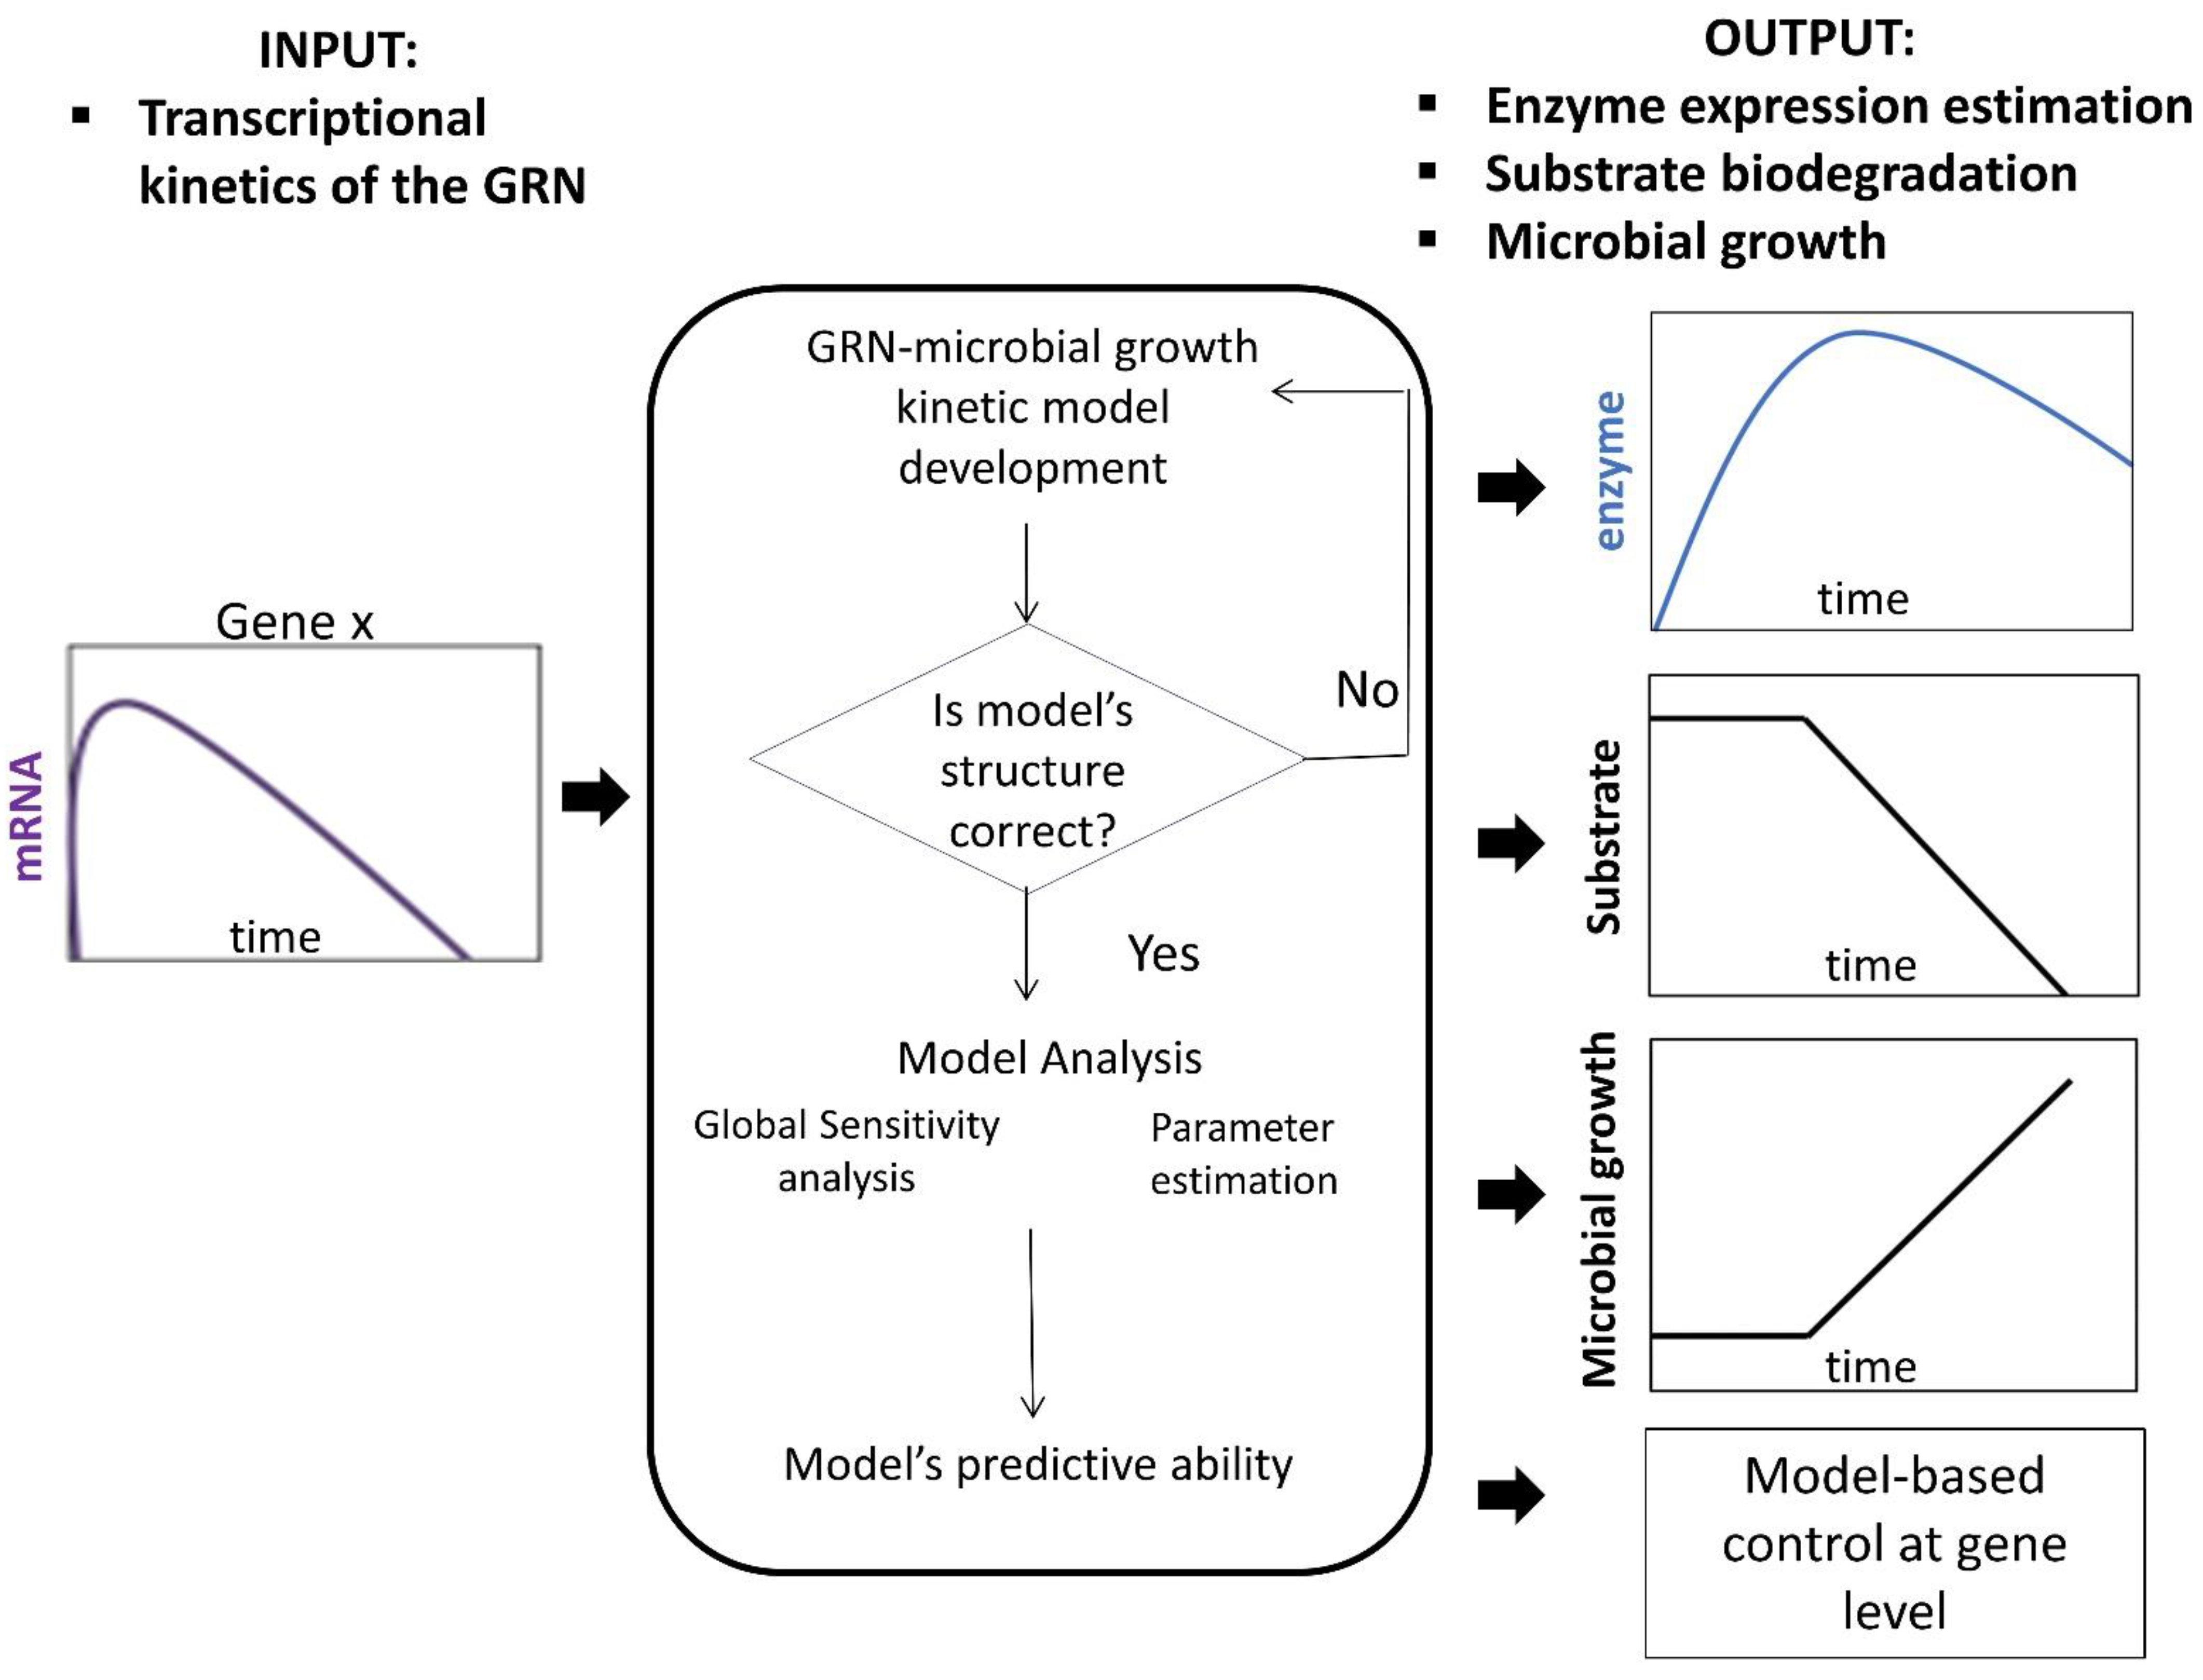
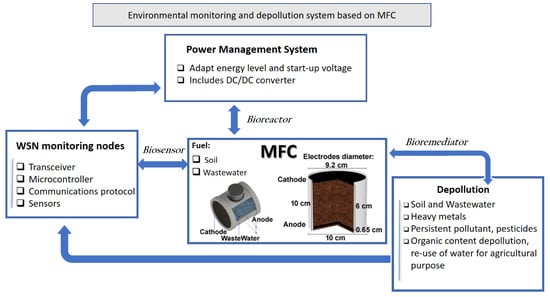
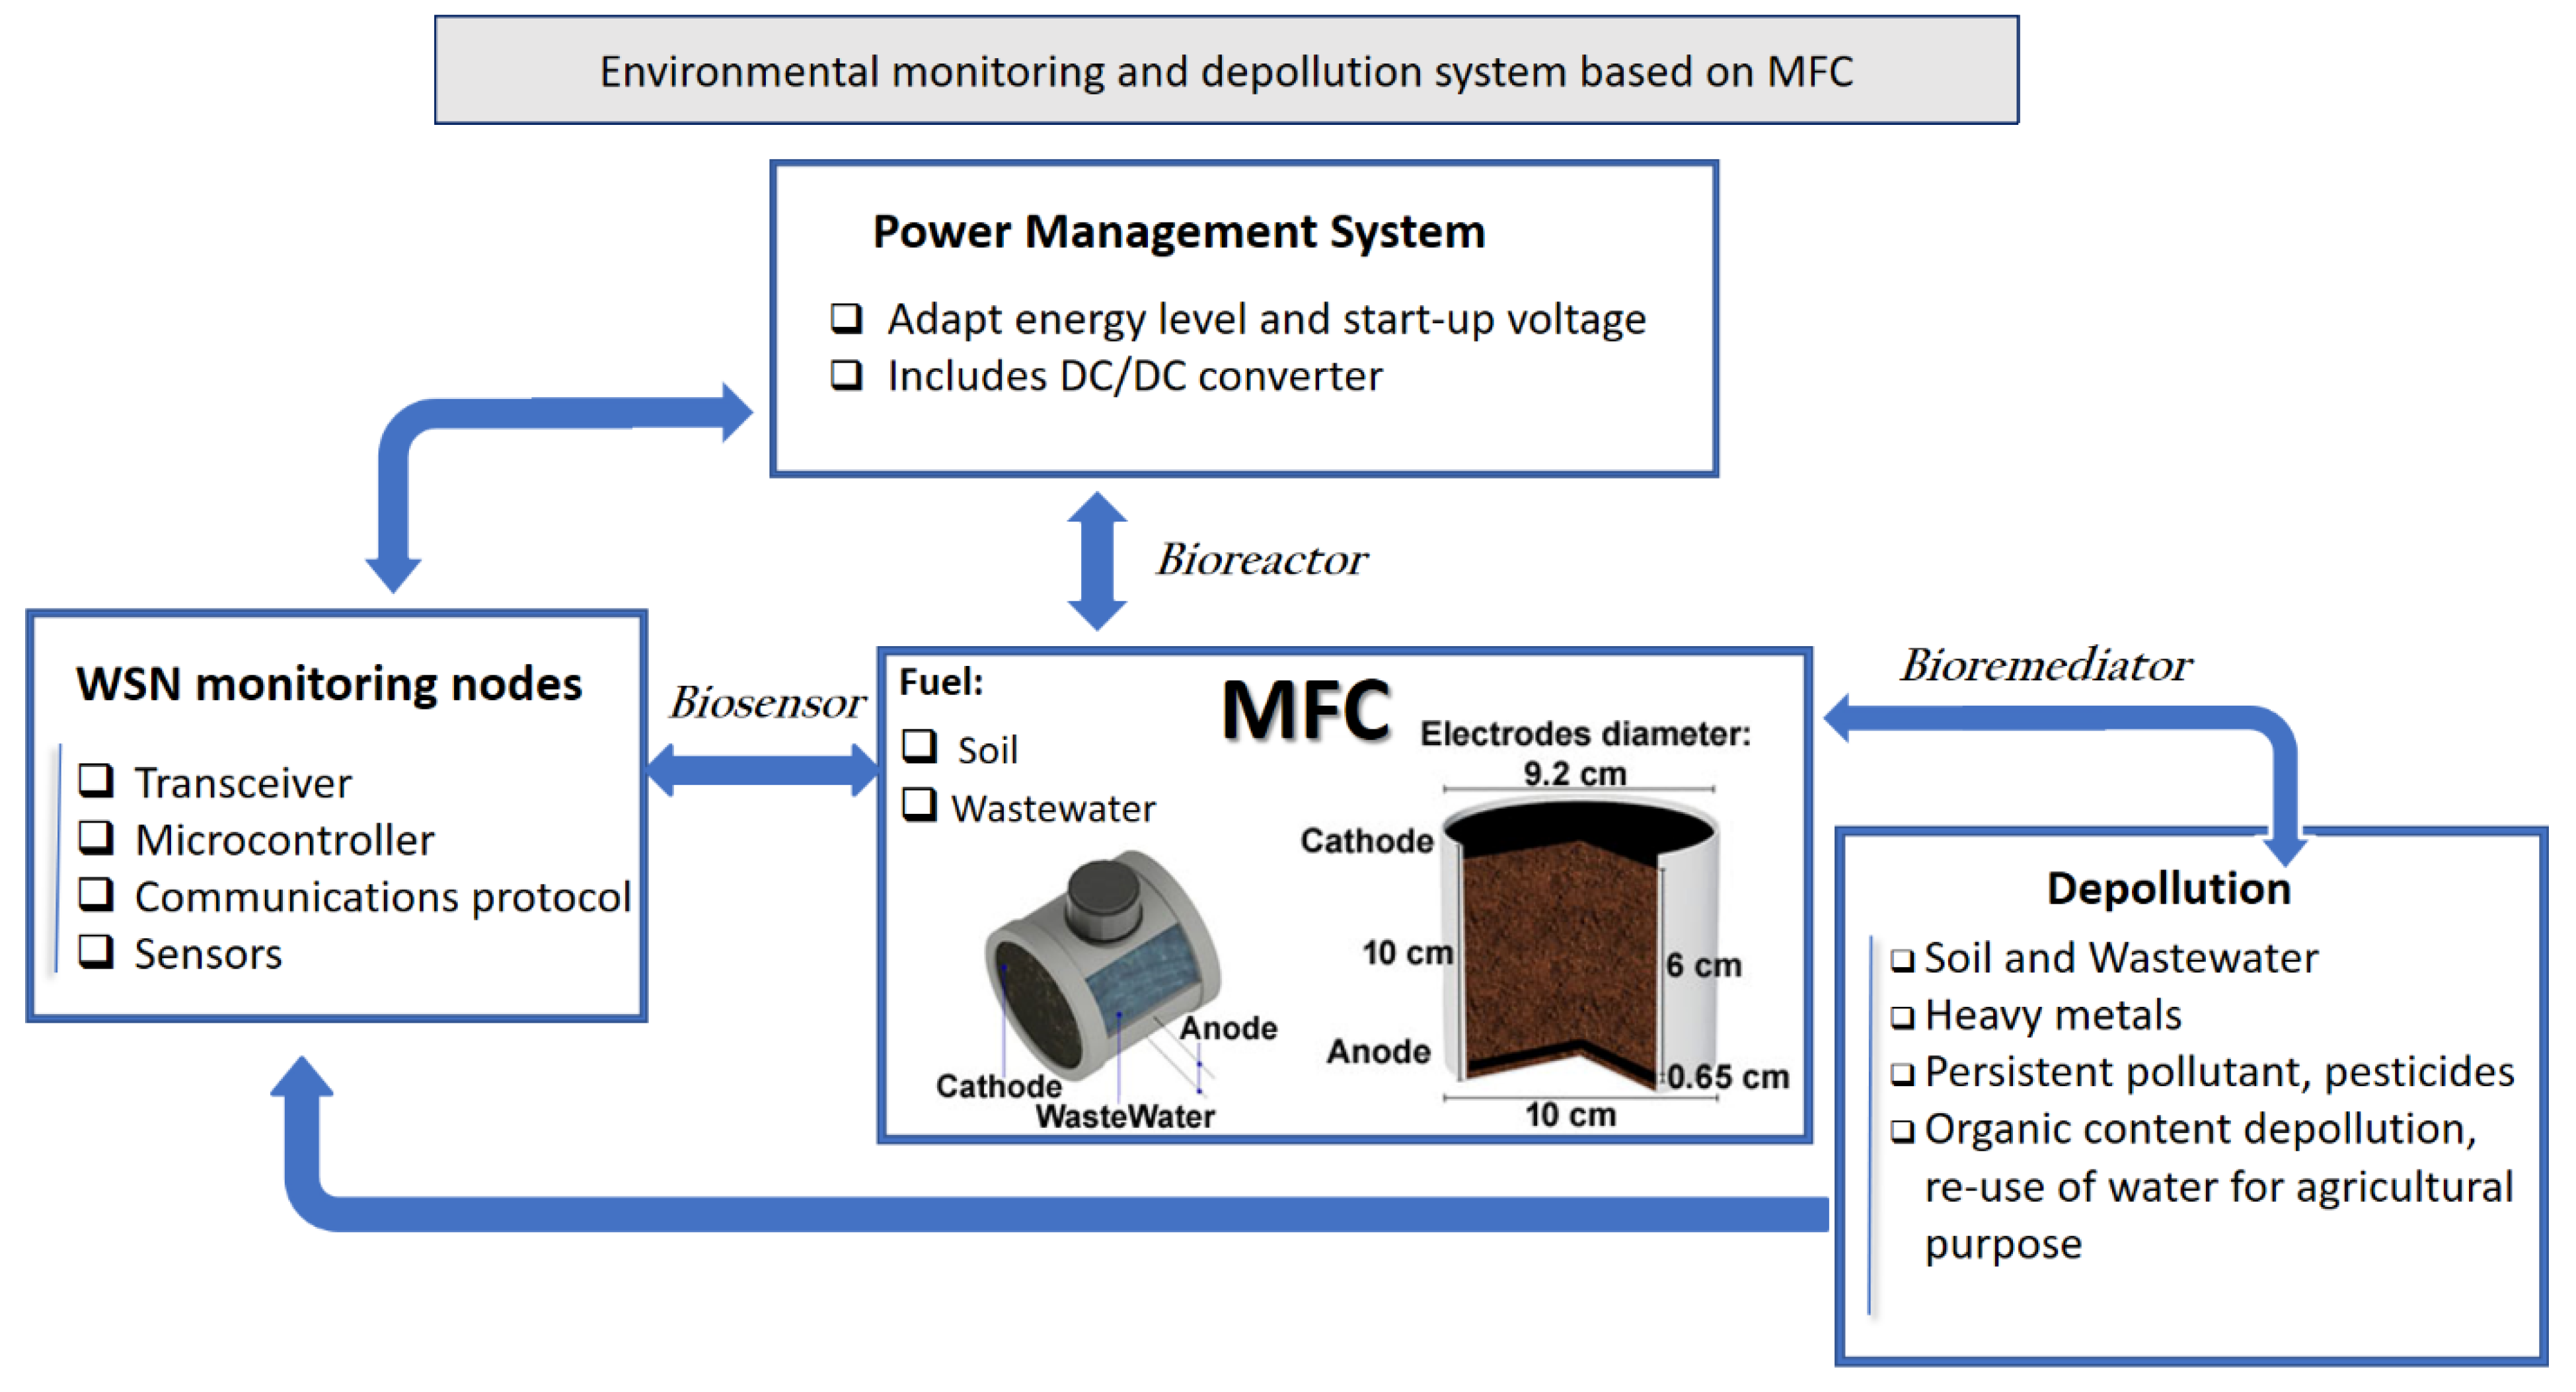

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2021 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).