


Abstract
Adaptive exposure to sub-lethal concentrations of sanitizers was previously reported to offer cross-protection to bacteria against antibiotics. This study was undertaken to determine whether the pre-exposure of fecal coliforms to suboptimal concentrations of a chemical sanitizer, chlorine dioxide (ClO2), alters their susceptibility to certain antibiotics. Fecal coliforms isolated from fresh fruit packing facilities (n = 12) were adapted in ½ or ¼ of the manufacturer-recommended concentration of ClO2. The susceptibility of the adapted and non-adapted cells to 13 different antibiotics was determined by observing the changes in their minimal inhibitory concentrations (MICs). The results showed that preadaptation to the suboptimal concentrations of ClO2, in general, either decreased or did not change the MICs of the antibiotics against selected fecal coliform isolates, with only two exceptions; preadaptation increased the MICs of kanamycin against two of the fecal coliform isolates, and of nalidixic acid against one of the fecal coliform isolates. The results suggest that the use of ClO2 has a relatively low risk of inducing the resistance of fecal coliforms to antibiotics.
1. Introduction
Chemical sanitizers are widely used in food production environments for the decontamination of food contact surfaces and the prevention of microbial contamination [1,2]. Russell [3] stated that frequent use of sanitizers may impose selective pressure and contribute to the emergence of resistant microorganisms in food environments. Each sanitizer used by food processors has the manufacturer’s recommended working concentration and treatment protocols [4]; for example, the use of 5 parts per million (ppm) of chlorine dioxide (ClO2) solution is recommended to disinfect hard, non-porous food contact surfaces [5]. The application of sanitizers at concentrations lower than those recommended may allow some bacterial cells to evade routine sanitization treatment [6]. Repeated exposure to sub-inhibitory concentrations of sanitizers has been shown to result in enhanced tolerance of some bacterial species to chloramphenicol, erythromycin, and ciprofloxacin [7,8,9]. Escherichia coli cells exposed to sub-inhibitory concentrations of benzalkonium chloride had elevated tolerance to chloramphenicol. The cells of Salmonella typhimurium that were pre-exposed to sub-inhibitory concentrations of acidified sodium chlorite had increased resistance to streptomycin, erythromycin, rifampicin, and chloramphenicol [10].
At present, a few reports have demonstrated cross-protection between clinically used antibiotics and ClO2, a chemical sanitizer commonly used by the food industry. Pre-exposure to the sanitizer rendered the cells of S. typhimurium able to tolerate an increased concentration of antibiotics [1]. However, opposite findings were reported in several other studies [10,11,12,13]. Pre-exposure to ClO2 either decreased or did not alter the susceptibility of Salmonella, E. coli, and Campylobacter cells to several antibiotics frequently used in human medicine. The objective of this study was to determine whether pre-exposure to suboptimal concentrations of ClO2 alters the susceptibility of selected fecal coliforms to the antibiotics used in human medicine.
2. Results
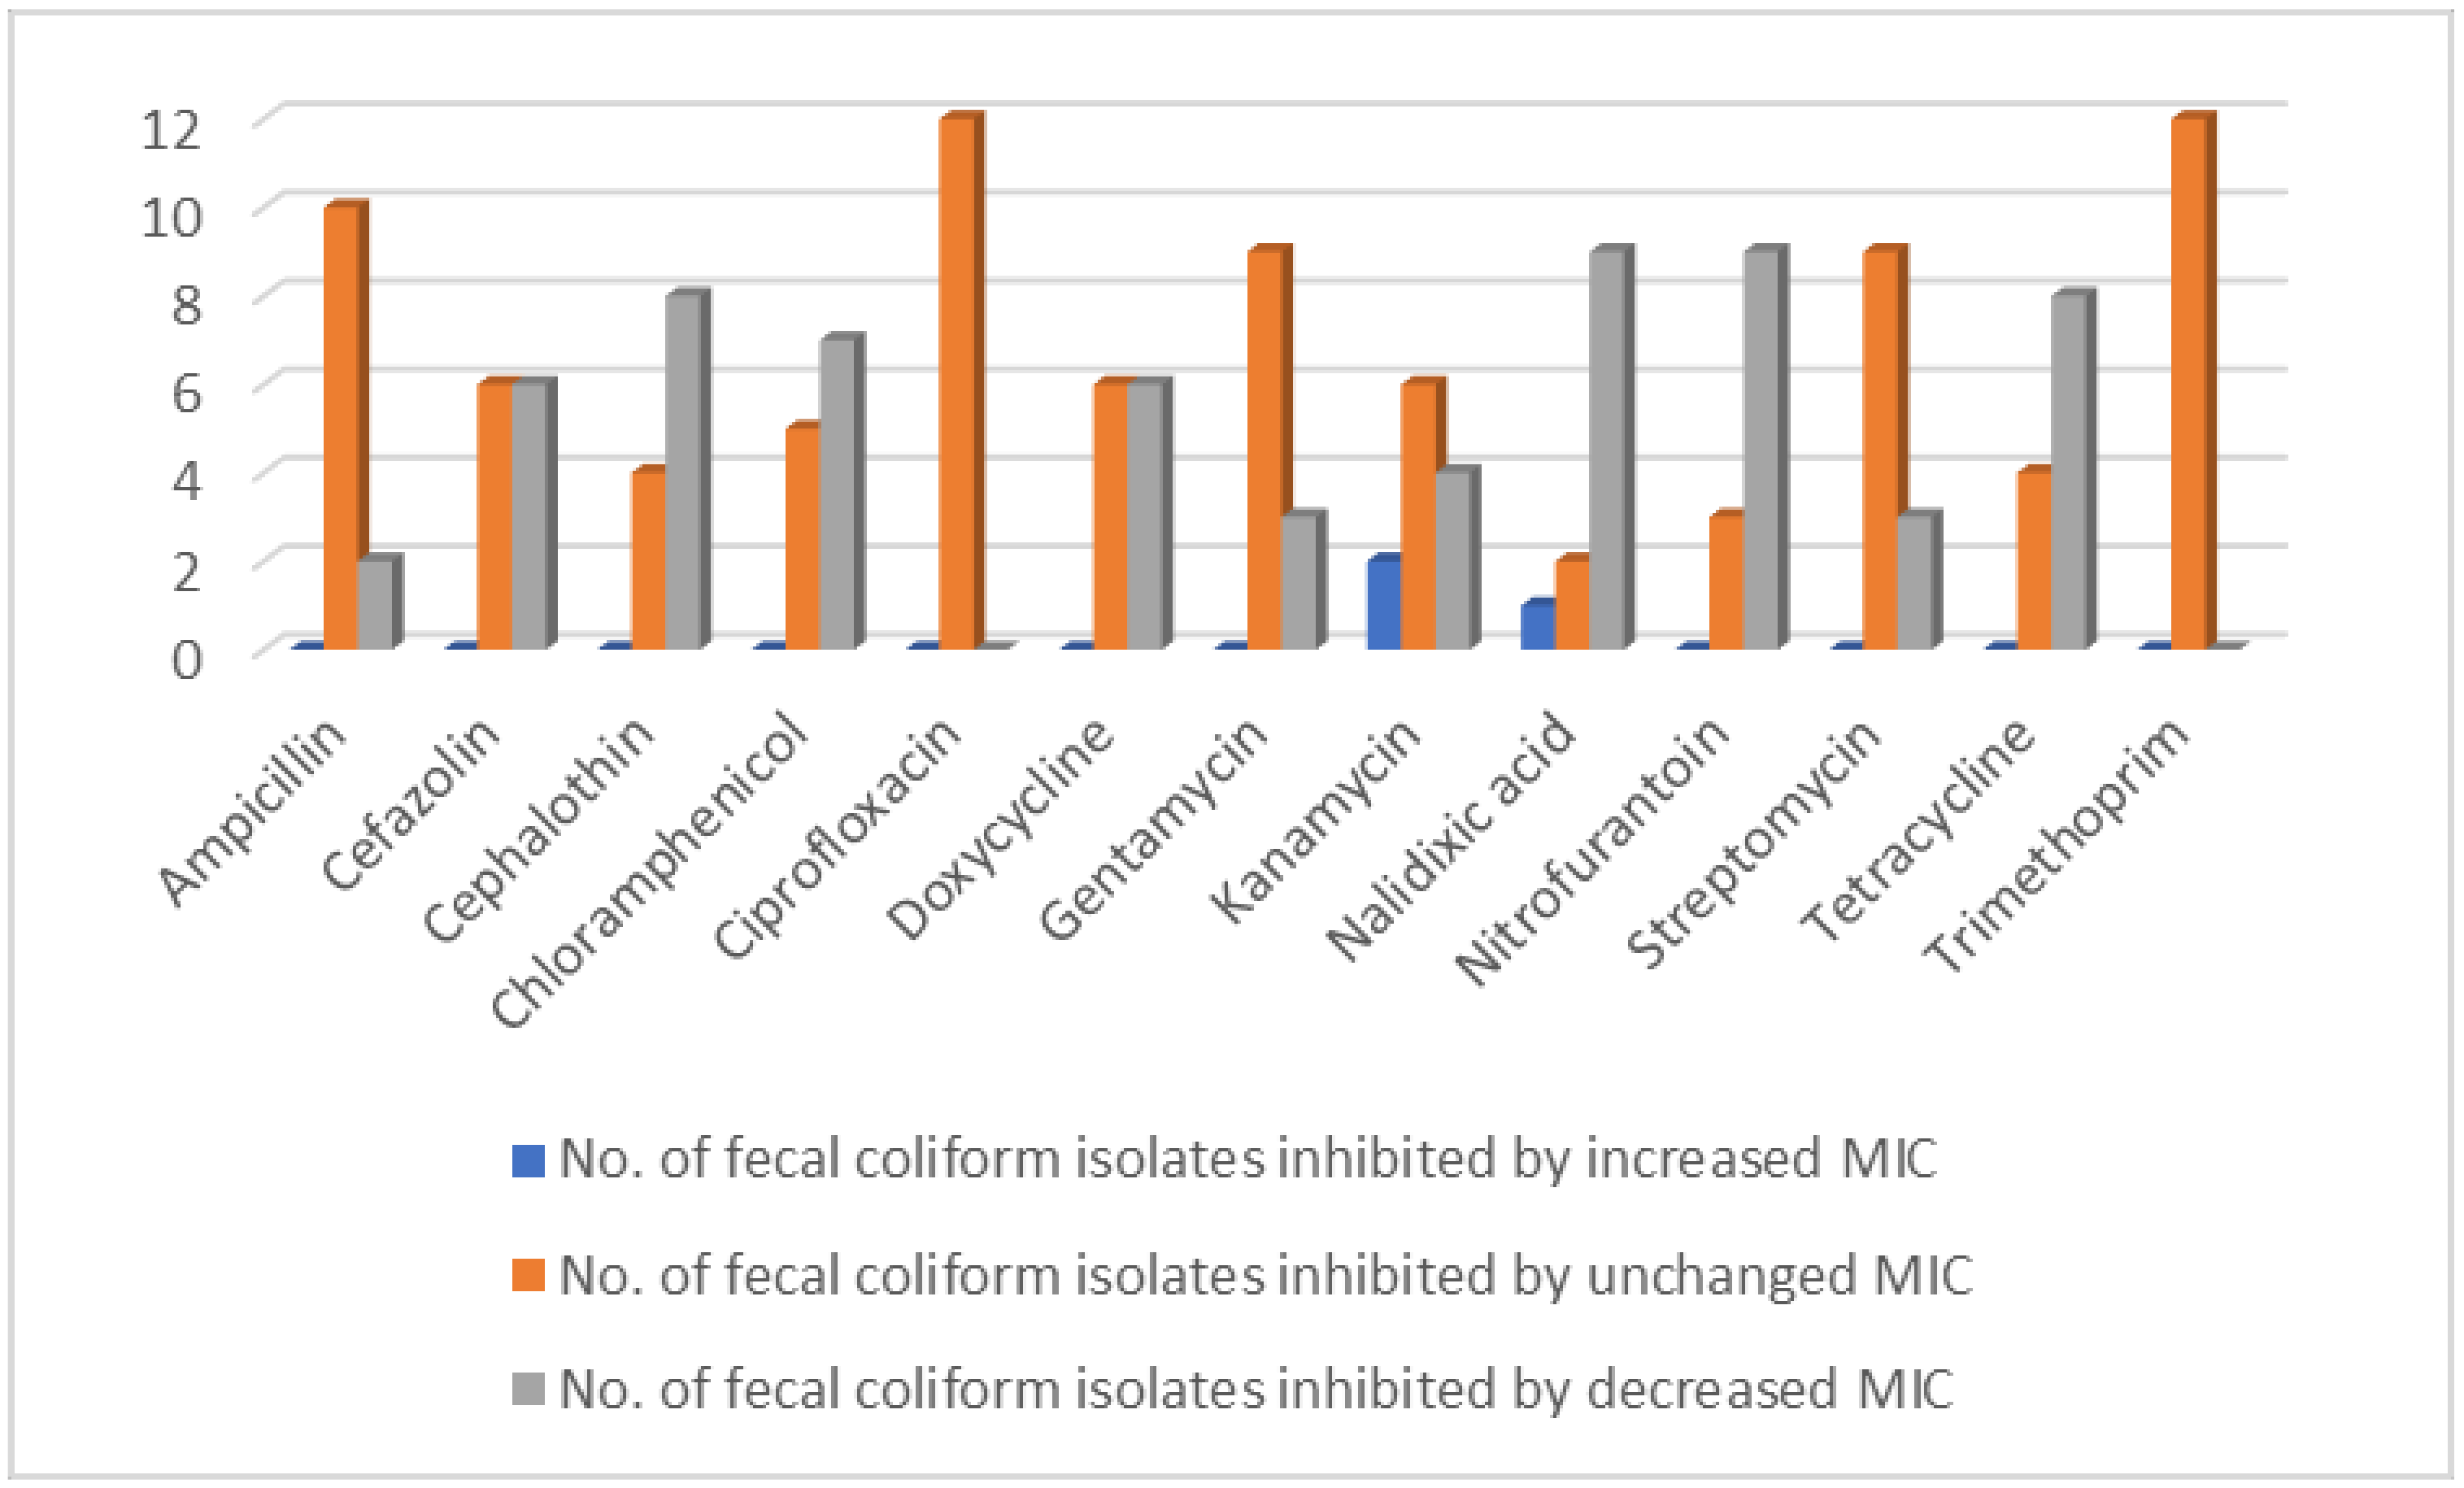
The minimum inhibitory concentrations (MICs) of selected antibiotics against fecal coliforms with or without preadaptation in suboptimal concentrations of ClO2 are shown in Table 1. The results suggest that the preadaptation process did not change the MICs of ciprofloxacin and trimethoprim against all twelve fecal coliform isolates used in the study (Figure 1).
Table 1.
Minimum inhibitory concentrations of various antibiotics against selected fecal coliforms preadapted in suboptimal concentrations of ClO2.
Figure 1.
The number of tested fecal coliform isolates completely inhibited by a changed or unchanged minimal inhibitory concentration of antibiotics.
A decrease in the MICs of cephalothin and tetracycline was observed with eight of the fecal coliform isolates, whilst the MICs against the other four fecal coliform isolates remained unchanged. A decrease in the MICs of gentamycin and streptomycin was observed with three of the fecal coliform isolates, and of cefazolin and doxycycline with six of the isolates, respectively, whilst the MICs remained the same for the rest of the fecal coliform isolates used in the study. The other three antibiotics, ampicillin, chloramphenicol, and nitrofurantoin, each had a decreased MIC against two, seven, and nine of the isolates used in this study, respectively. However, preadaptation with sub-lethal concentrations of ClO2 increased the MICs of kanamycin against two of the fecal coliform isolates, and decreased the MICs against four of the fecal coliform isolates. The MIC of nalidixic acid increased for one of the fecal coliform isolates and decreased for nine of the fecal coliform isolates.
The susceptibility of selected fecal coliforms to various antibiotics, as affected by preadaptation in suboptimal concentrations of ClO2, is shown in Table 2.
Table 2.
Changes in the susceptibility of selected fecal coliforms to various antibiotics, as affected by preadaptation in sub-lethal concentrations of ClO2.
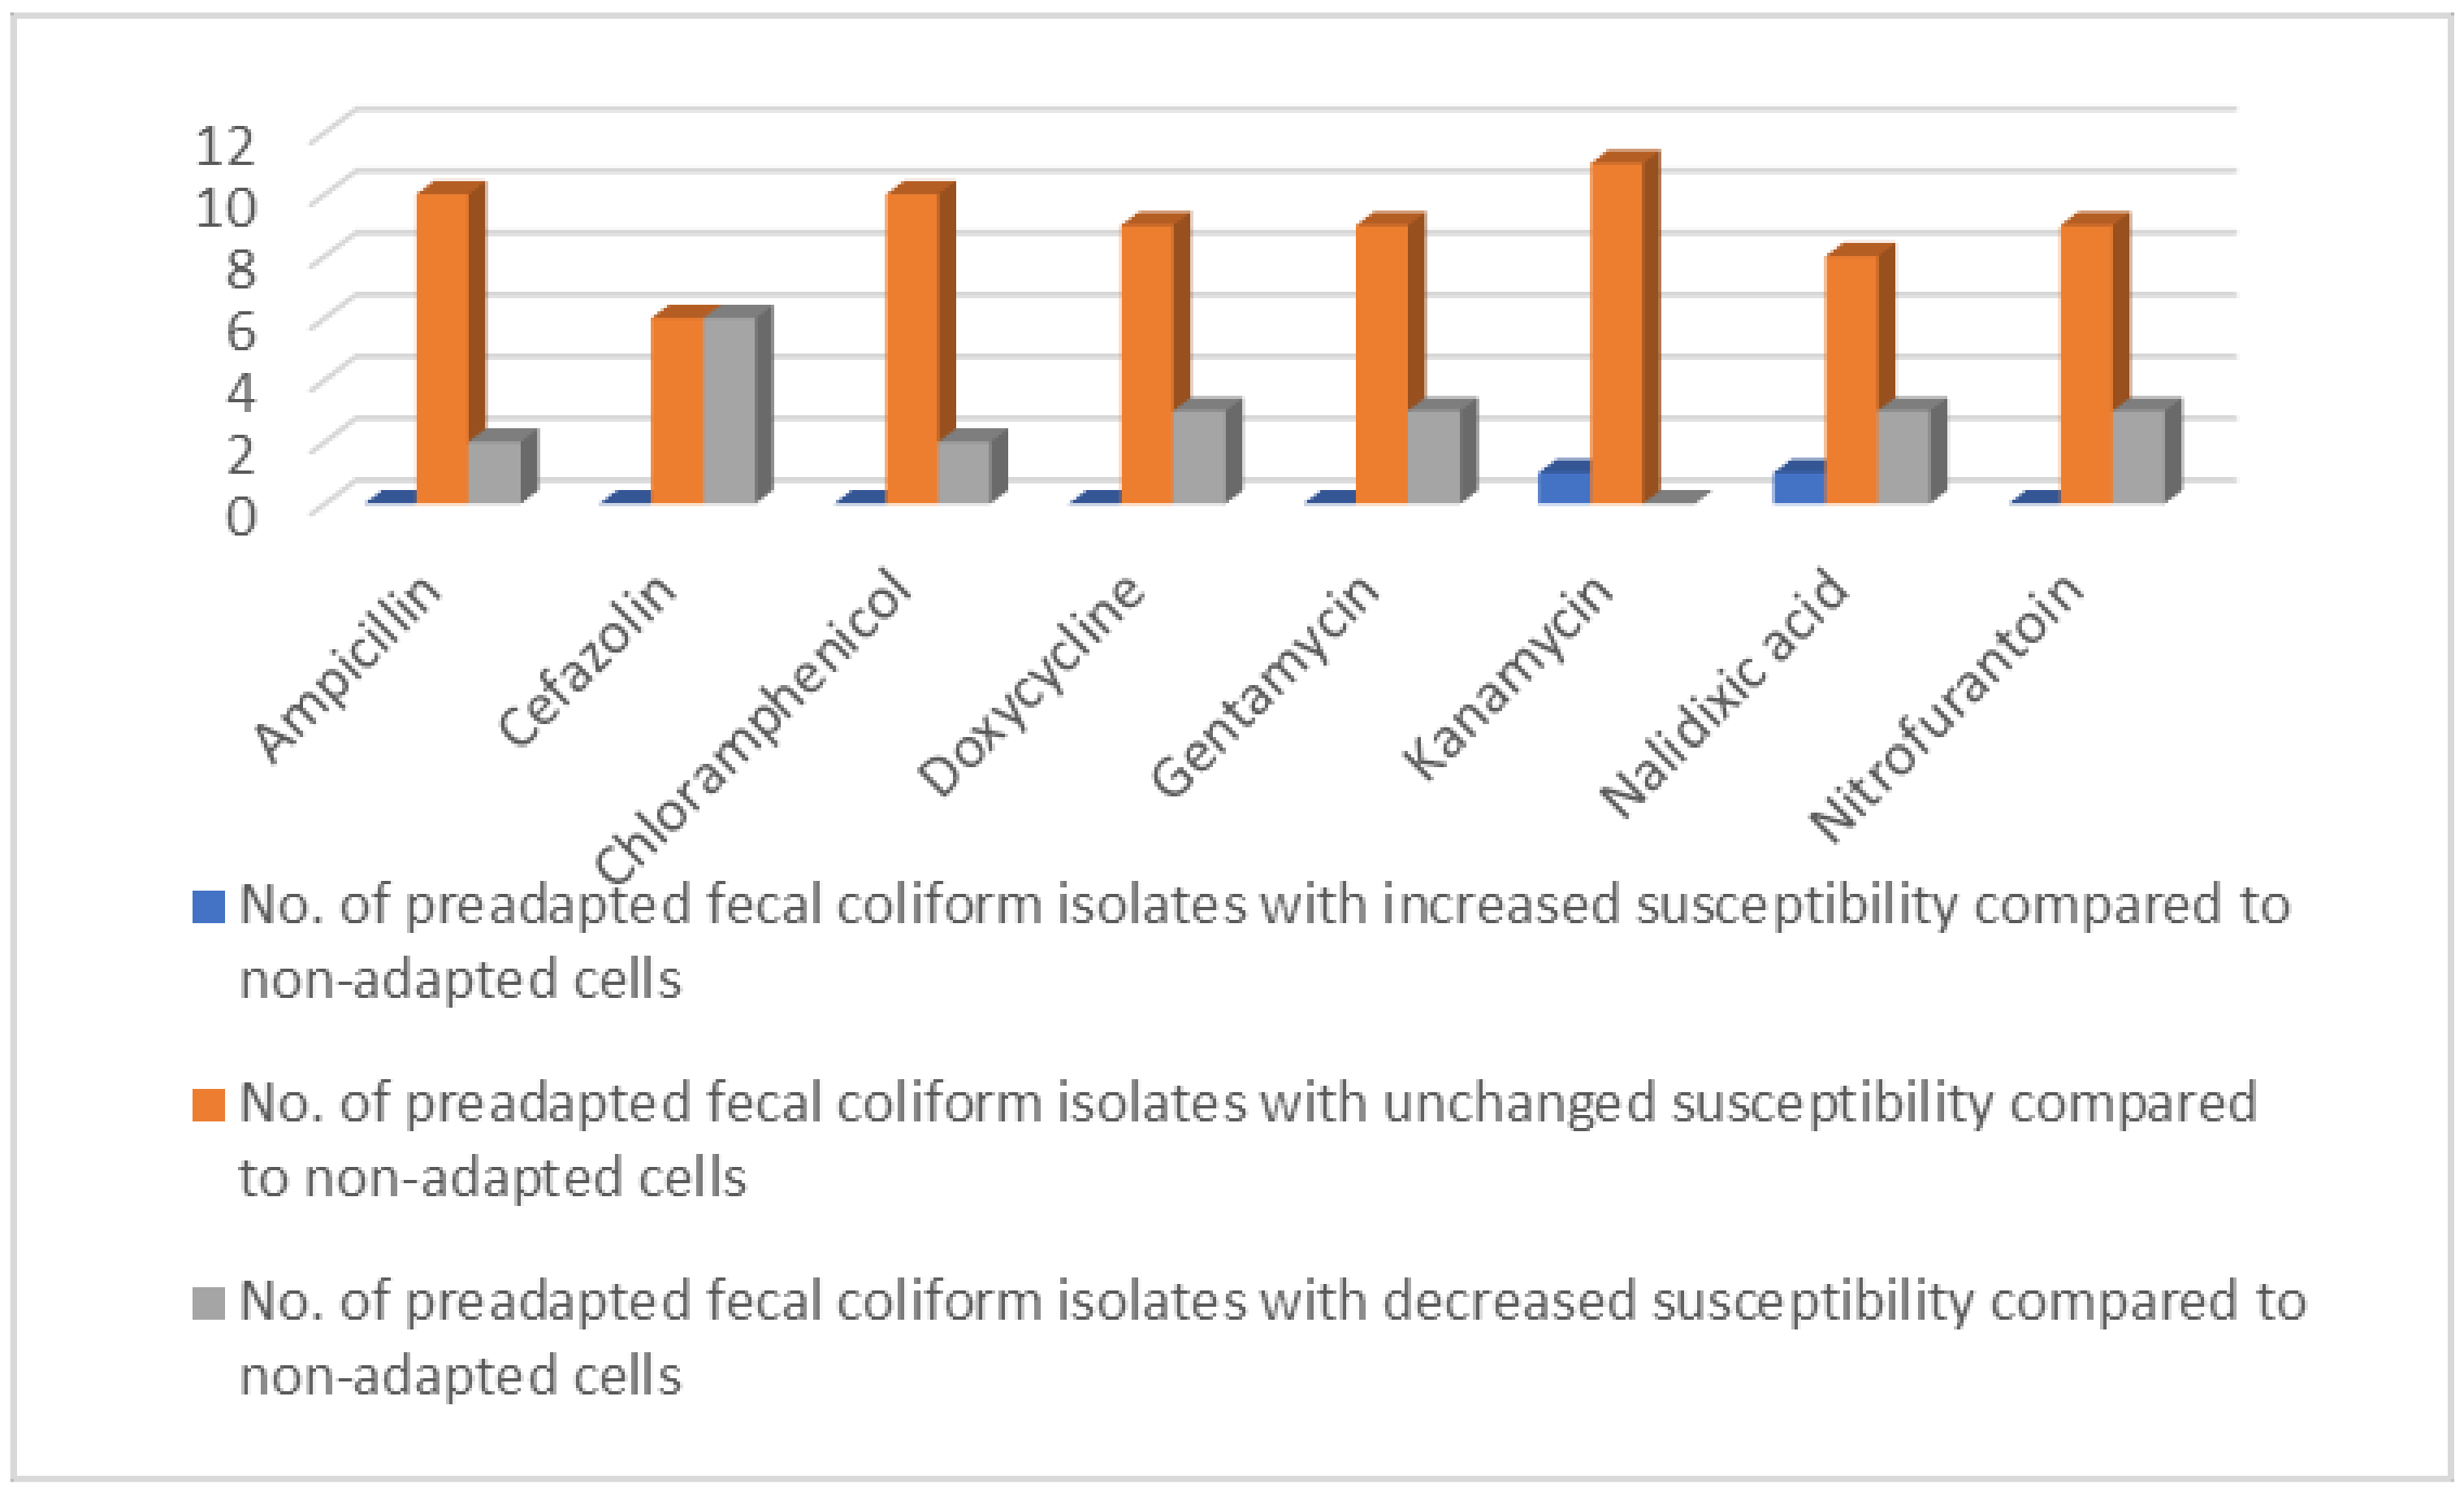
It was observed that the preadaptation process, in the vast majority of cases, either did not change or decreased the susceptibility of the fecal coliforms to the tested antibiotics, changing from resistant/intermediate resistant to intermediate resistant/sensitive (Figure 2).
Figure 2.
The number of preadapted fecal coliform isolates with changed or unchanged susceptibility to various antibiotics, compared to non-adapted cells, according to the breakpoints. Preadaptation did not change the MICs of ciprofloxacin, streptomycin, and trimethoprim, and these antibiotics are excluded from the figure.
The increase in MIC only changed the susceptibility of two fecal coliform isolates from sensitive to resistant/intermediate resistant, one to kanamycin and another to nalidixic acid.
3. Discussion
In this study, it was observed that the MICs of some of the antibiotics against certain fecal coliform isolates were unchanged or decreased by the preadaptation treatments in two different suboptimal concentrations of ClO2 (Table 1 and Figure 1). Similarly, preadaptation either did not change or decreased the susceptibility of some of the fecal coliform isolates to the evaluated antibiotics (Table 2 and Figure 2). Consistent with the results of the present study, Alonso-Hernando et al. [10] reported that the preadaptation of S. enteritidis in ClO2 did not change its susceptibility to gentamicin, amoxicillin–clavulanic acid, ciprofloxacin, and tetracycline. The pre-exposure of Salmonella and Campylobacter to ClO2 did not change their susceptibility to ampicillin, chloramphenicol, ciprofloxacin, gentamicin, kanamycin, nalidixic acid, streptomycin, tetracycline, and trimethoprim/sulfamethoxazole [11]. The exposure of E. coli to sub-inhibitory concentrations of another oxidizing sanitizer, sodium hypochlorite, did not change its susceptibility to several antibiotics, including ampicillin, gentamicin, and ciprofloxacin [12]. Soumet et al. [13] observed that the pre-exposure of E. coli to a quaternary ammonium cation led to a four-fold decrease in the MICs of ciprofloxacin, nalidixic acid, trimethoprim, and ampicillin. These phenomena can be explained by the mechanistic variances in the effect of ClO2 vs. the evaluated antibiotics on bacterial cells, or by the differences in the location and regulation of the genes encoding bacterial resistance against the two different types of antimicrobial agents [14].
Treatment with a lower ClO2 concentration than that recommended by the manufacturer may not kill fecal coliform bacterial cells, but likely exerts sub-lethal injuries to them. Sub-lethal injuries have been reported to cause increased, or even newly developed, sensitivity of damaged cells to selective agents in microbiological media [15,16], as well as antimicrobials or similar substances; for example, sub-lethal treatments have made some bacterial pathogens lose their tolerance to salt, increase their susceptibility to deoxycholate, and become sensitive to sodium azide.
Other than enhanced susceptibility to selective agents used in microbiological media and other antimicrobials, cellular modifications, such as the leakage of intracellular materials and modified metabolic activities, have also been observed in sub-lethally injured bacterial cells [17]. Oxidizing agents, such as ClO2, generate hydroxy radicals, which may interfere with the activity of intracellular enzymes and the metabolic pathways in microbial cells, which could lead to decreased susceptibility to antibiotics [18]. ClO2 also inhibits the activity of cell membrane proteins, increasing the permeability of the outer and cytoplasmic membranes [19]. Loss of integrity of the cytoplasmic membrane may lead to more effective intake of antibiotics and, eventually, increased susceptibility of bacterial cells to antibiotics [20].
In the current study, preadaptation with sub-lethal concentrations of ClO2 increased the MICs of kanamycin against two of the fecal coliform isolates, and the MIC of nalidixic acid against one of the fecal coliform isolates (Table 1 and Figure 1). In a previous study, repeatedly exposing the cells of a poultry isolate of S. typhimurium to increasing sub-lethal concentrations of ClO2 resulted in a 1.13-fold increase in the MIC of streptomycin compared to unexposed cells [1]. When bacteria cells were pretreated with chlorhexidine, resistance to ceftazidime, sulfamethoxazole, imipenem, cefotaxime, and tetracycline was induced [7,21,22,23]. The mechanism of cross-protection between ClO2 and antibiotics has not yet been determined. It has been suggested that the possible linkage between resistance to antibiotics and sanitizers might be due to common resistance mechanisms, such as the involvement of multidrug efflux pumps [15] and the production of stress response proteins [24].
It is worth noting that this study evaluated the in vitro MICs of various antibiotics against selected bacterial isolates. It is not known whether the results have any relevance from a biological or clinical standpoint.
4. Materials and Methods
Cells of fecal coliform bacteria (n = 12), F5, F8, F35, F252, F219, F112, F272, F174, F329, F354, F390, and F406, previously isolated from fresh produce packing facilities in a separate research project of our laboratory [25], were used in this study. According to the results of 16S rDNA sequencing, they belong to the genus Klebsiella, Enterobacter, Pantoea, or Raoultella (Table 3) [26]. The isolates were retrieved from frozen storage and sub-cultured twice on tryptic soy agar (Becton Dickinson, Franklin Lakes, NJ) at 37 °C for 24 h. A single colony of each fecal coliform culture was transferred to 9 mL Mueller–Hinton (MH) broth (Becton Dickinson), and the broth cultures were incubated at 37 °C for 16 h.
Table 3.
Identities of the bacterial isolates used in the study.
A commercial, ClO2-generating product, Selectrocide-2L500-(Selective Micro Technologies, Dublin, OH, USA), was used to generate chlorine dioxide in this study. The product arrived in solid form and produced 2 L of 500 ppm ClO2 solution when activated by the addition of sterile distilled water. The activated product was diluted on the day of the experiment to a working concentration of 5 or 2.5 ppm with sterile distilled water.
The fecal coliform cultures described above were diluted to 105 CFU/mL using a double-strength MH broth, and each diluted culture was then mixed with an equal volume of the 5 or 2.5 ppm ClO2 solution with a vortex, generating a fecal coliform cell suspension in a single-strength MH broth containing 2.5 or 1.25 ppm ClO2. The fecal coliform cells were adapted in the MH broth with the suboptimal concentrations of ClO2 at room temperature for 1 min before being mixed with an equal volume of Dey–Engley (DE) neutralizing broth (Becton Dickinson). The MICs of the adapted and non-adapted cells of the fecal coliforms were determined using the protocols described below.
To obtain the MICs, adapted and non-adapted cells of each fecal coliform culture in the DE neutralizing broth were centrifuged for 5 min at 4200× g. The supernatant was removed, and the cell pellet was rinsed twice with sterile deionized water. After the final wash, 0.5 mL of each bacterial cell suspension in sterile deionized water was added into a series of 4.5 mL of MH broth containing an appropriate concentration (2-fold dilution series from 2 to 256 µg/mL) of each of the 13 antibiotics, including ampicillin, cefazolin, cephalothin, chloramphenicol, ciprofloxacin, doxycycline, gentamicin, kanamycin, nalidixic acid, nitrofurantoin, streptomycin, tetracycline, and trimethoprim (Oxoid Ltd., Basingstoke, Hants, UK). The MH broth with the inoculated fecal coliforms was incubated at 37 °C for 16–20 h. The lowest concentration of an antibiotic that inhibited the growth of the bacterial cells after overnight incubation was regarded as the MIC. The MICs of the antibiotics for the sanitizer-adapted and non-adapted cells of fecal coliforms were compared. Susceptibility categorization was assessed according to the current susceptibility and resistant breakpoints advised by the Clinical and Laboratory Standards Institute [27]. Each experiment was conducted in two independent trials.
5. Conclusions
This study investigated the changes in antibiotic resistance of selected fecal coliform bacteria after being preadapted with sub-lethal concentrations of ClO2. Most fecal coliform bacteria used in the study demonstrated either the same or reduced resistance to the evaluated antibiotics, but slightly stronger resistance to nalidixic acid and kanamycin was demonstrated by one to two of the fecal coliform isolates. The results suggest that the use of ClO2 had a relatively low risk of inducing fecal coliform resistance to antibiotics.
Author Contributions
Conceptualization, J.C.; methodology, J.C. and H.G.; formal analysis, H.G.; data curation, H.G.; writing—original draft preparation, H.G. and J.Q.; writing—review and editing, J.C., D.L. and J.Q.; supervision, J.C.; project administration, J.C.; funding acquisition, J.C. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by the National Institute of Food and Agriculture, U.S. Department of Agriculture, under award number USDA-NIFA-SCRI-004530.
Data Availability Statement
Data are contained within the article.
Conflicts of Interest
The authors declare no conflict of interest. The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript, or in the decision to publish the results.
References
- Espina, L.; García-Gonzalo, D.; Pagán, R. Detection of Thermal Sublethal Injury in Escherichia coli via the Selective Medium Plating Technique: Mechanisms and Improvements. Front. Microbiol. 2016, 7, 1376. [Google Scholar] [CrossRef] [Scilit]
- Ikai, H.; Odashima, Y.; Kanno, T.; Nakamura, K.; Shirato, M.; Sasaki, K.; Niwano, Y. In Vitro Evaluation of the Risk of Inducing Bacterial Resistance to Disinfection Treatment with Photolysis of Hydrogen Peroxide. PLoS ONE 2013, 8, e81316. [Google Scholar] [CrossRef] [Scilit]
- Mavri, A.; Možina, S.S. Development of antimicrobial resistance in Campylobacter jejuni and Campylobacter coli adapted to biocides. Int. J. Food Microbiol. 2012, 160, 304–312. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Condell, O.; Iversen, C.; Cooney, S.; Power, K.A.; Walsh, C.; Burgess, C.; Fanning, S. Efficacy of Biocides Used in the Modern Food Industry to Control Salmonella enterica, and Links between Biocide Tolerance and Resistance to Clinically Relevant Antimicrobial Compounds. Appl. Environ. Microbiol. 2012, 78, 3087–3097. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Møretrø, T.; Høiby-Pettersen, G.S.; Habimana, O.; Heir, E.; Langsrud, S. Assessment of the antibacterial activity of a triclosan-containing cutting board. Int. J. Food Microbiol. 2011, 146, 157–162. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Araújo, P.; Lemos, M.; Mergulhão, F.; Melo, L.; Simões, M. Antimicrobial resistance to disinfectants in biofilms. In Science against Microbial Pathogens: Communicating Current Research and Technological Advances, 1st ed.; Méndez-Vilas, A., Ed.; Formatex Research Center: Badajoz, Spain, 2011; pp. 826–834. [Google Scholar]
- Borges-Walmsley, M.I.; McKeegan, K.S.; Walmsley, A.R. Structure and function of efflux pumps that confer resistance to drugs. Biochem. J. 2003, 376, 313–338. [Google Scholar] [CrossRef] [Scilit]
- Clinical and Laboratory and Standards Institute. Performance Standards for Antimicrobial Susceptibility Testing, 27th ed.; Clinical and Laboratory and Standards Institute: Wayne, PA, USA, 2017. [Google Scholar]
- IFT. Antimicrobial resistance: Implications for the food system. Compr. Rev. Food Sci. Food Saf. 2006, 5, 71–137. [Google Scholar] [CrossRef] [Scilit]
- Alonso-Hernando, A.; Capita, R.; Prieto, M.; Alonso-Calleja, C. Comparison of antibiotic resistance patterns in Listeria monocytogenes and Salmonella enterica strains pre-exposed and exposed to poultry decontaminants. Food Control 2009, 20, 1108–1111. [Google Scholar] [CrossRef] [Scilit]
- Berrang, M.E.; Meinersmann, R.J.; Cox, N.A.; Cray, P. Application of chlorine dioxide to lessen bacterial contamination during broiler defeathering. J. Appl. Poult. Res. 2011, 20, 33–39. [Google Scholar] [CrossRef] [Scilit]
- Busta, F.F. Practical Implications of Injured Microorganisms in Food. J. Milk Food Technol. 1976, 39, 138–145. [Google Scholar] [CrossRef] [Scilit]
- Nikaido, H. Multidrug efflux pumps of gram-negative bacteria. J. Bacteriol. 1996, 178, 5853–5859. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gadea, R.; Fernández Fuentes, M.A.; Pérez Pulido, R.; Gálvez, A.; Ortega, E. Effects of exposure to quater-nary-ammonium-based biocides on antimicrobial susceptibility and tolerance to physical stresses in bacteria from organic foods. Food Microbiol. 2017, 63, 58–71. [Google Scholar] [CrossRef] [Scilit]
- Davin-Regli, A.; Pagés, J.M. Cross-resistance between biocides and antimicrobials: An emerging question. OIE Rev. Sci. Tech. 2012, 31, 89–104. [Google Scholar] [CrossRef] [Scilit]
- Piddock, L.J.V. Multidrug-resistance efflux pumps? Not just for resistance. Nat. Rev. Genet. 2006, 4, 629–636. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Braoudaki, M.; Hilton, A.C. Adaptive Resistance to Biocides in Salmonella enterica and Escherichia coli O157 and Cross-Resistance to Antimicrobial Agents. J. Clin. Microbiol. 2004, 42, 73–78. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hricova, D.; Stephan, R.; Zweifel, C. Electrolyzed Water and Its Application in the Food Industry. J. Food Prot. 2008, 71, 1934–1947. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Levy, S.B. Active efflux, a common mechanism for biocide and antibiotic resistance. J. Appl. Microbiol. 2002, 92, 65–71. [Google Scholar] [CrossRef] [Scilit]
- Cruz, C.D.; Fletchr, G.C. Assessing manufacturers’ recommended concentrations of commercial sanitizers on inactivation of Listeria monocytogenes. Food Control 2012, 26, 194–199. [Google Scholar] [CrossRef] [Scilit]
- Delcour, A.H. Outer membrane permeability and antibiotic resistance. Biochim. Biophys. Acta Proteins Proteom. 2009, 1794, 808–816. [Google Scholar] [CrossRef] [Scilit]
- Ofori, I.; Maddila, S.; Lin, J.; Jonnalagadda, S.B. Chlorine dioxide oxidation of Escherichia coli in water—A study of the disinfection kinetics and mechanism. J. Environ. Sci. Health 2017, 52, 598–606. [Google Scholar] [CrossRef] [Scilit]
- Poole, K.; Srikumar, R. Multidrug efflux in Pseudomonas aeruginosa: Components, mechanisms and clinical significance. Curr. Top. Med. Chem. 2001, 1, 59–71. [Google Scholar] [CrossRef] [Scilit]
- Russel, A.D. A review: Plasmids and bacterial resistance to biocides. J. Appl. Microbiol. 1997, 82, 155–165. [Google Scholar] [CrossRef] [Scilit]
- Gazula, H.; Quansah, J.; Allen, R.; Scherm, H.; Li, C.; Takeda, F.; Chen, J. Microbial loads on selected fresh blueberry packing lines. Food Control 2019, 100, 315–320. [Google Scholar] [CrossRef] [Scilit]
- Gazula, H.; Scherm, H.; Li, C.; Takeda, F.; Wang, P.; Chen, J. Ease of biofilm accumulation, and efficacy of sanitizing treatments in removing the biofilms formed, on coupons made of materials commonly used in blueberry packing environment. Food Control 2019, 104, 167–173. [Google Scholar] [CrossRef] [Scilit]
- Capita, R.; Riesco-Peláez, F.; Alonso-Hernando, A.; Alonso-Calleja, C. Exposure of Escherichia coli ATCC 12806 to Sublethal Concentrations of Food-Grade Biocides Influences Its Ability to Form Biofilm, Resistance to Antimicrobials, and Ultrastructure. Appl. Environ. Microbiol. 2014, 80, 1268–1280. [Google Scholar] [CrossRef] [Scilit]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).