


Abstract
The aim of the study was to determine the effect of Fe glycine chelate supplementation on the chemical composition and nutritional quality of breast meat from broiler chicken. The following parameters were assessed: fat content, cholesterol content, fatty acid profile, atherogenic index (AI), thrombogenic index (TI), and hypocholesterolemic/hypercholesterolemic (H/H) fatty acid ratio. The 42-day experiment involved 200 broiler chickens assigned into four dietary groups: the control receiving Fe sulfate in the dose of 40 mg/kg of feed and three experimental groups of chickens supplemented with 40 mg (Fe-Gly40), 20 mg (Fe-Gly20), or 10 mg (Fe-Gly10) of Fe glycine chelate per 1 kg of diet. The results showed no negative effect of the application of Fe glycine chelate on the chemical composition and nutritional quality of breast muscle. Therefore, the advisability of the application of Fe glycine chelates in the nutrition of broiler chickens should be revised.
1. Introduction
Given the high content of polyunsaturated fatty acids (PUFAs), particularly the n − 3 family, and the low content of fat and cholesterol, poultry meat is regarded to have high dietary value and bring much more beneficial effects on consumer health than red meat [1,2]. Investigations conducted by our research team and other researchers have demonstrated that the dietary quality of poultry meat can be modified through alterations in broiler chicken nutrition. For instance, supplementation with PUFAs, herbs, and minerals used as easily assimilable organic compounds has been found to be effective [3,4,5,6,7,8].
Iron (Fe) plays an important role in all living organisms. It has an impact on hematopoietic processes, oxygen and electron transport, DNA synthesis, and immunity. In turn, the deficiency of this element worsens animal health status [9,10]. Fe exhibits antioxidant activity (e.g., it is part of catalase; each of the catalase subunits contains a heme system with a central iron atom); however, since Fe is a catalyst of PUFA oxidation, its excessive supply may have a pro-oxidative effect [11]. Hence, it is important to provide appropriate dietary amounts of Fe tailored to the needs of chickens. Additionally, research results highlight the importance of the form of Fe administered to chickens, as it has been shown that organic forms have a positive effect on Fe assimilation [12]. In turn, due to the presence of ferritin, the level of Fe in the organism has an impact on Fe and lipid (including cholesterol) pathways and may modify the content of these components in meat [13]. Iron is present in the cytochrome and terminal components of stearoyl coenzyme A (CoA) desaturase, which converts palmitic acid (16:0) to palmitoleic acid (16:ln-7) and stearic acid (18:0) to oleic acid (18:ln-9) [14]. It has also been shown that Fe deficiency may have an impact on the activity or synthesis of A6-desaturase and thus alter PUFA metabolism and tissue composition. In the biosynthesis of long-chain PUFAs, desaturases catalyze the insertion of a double bond in the cis configuration between carbon atoms of active fatty acids. This reaction involves the transfer of an electron by NADH reductase to cytochrome b5, whose active center contains two non-heme iron atoms [14]. The aim of the present study was to assess the possible effect of Fe glycine chelate applied in feed rations for Ross 308 broiler chickens on the nutritional quality of the breast muscle of these birds. More specifically, the total fat and cholesterol content as well as the fatty acid profile with its indicators, i.e., the atherogenic index (AI), the thrombogenic index (TI), and the hypocholesterolemic/hypercholesterolemic (H/H) fatty acid ratio, were determined.
2. Materials and Methods
All procedures were used in the experiment in compliance with the consent from the Local Bioethics Committee for experimental animals, University of Life Sciences in Lublin, Poland (Resolution No. 37/2011 of 17 May 2011).
2.1. Experimental Factor
Previous investigations carried out by our team demonstrated that supplementation of the diet for Ross 308 chickens with Fe glycine chelate at the doses of 40, 20, or 10 mg/kg of feed (covering 100%, 50%, or 25% of the demand) increased the efficiency of chicken fattening, lowered the percentage of chicken falls, and stimulated cellular defense mechanisms (increased percentage of T1 helper cells and enhanced production of cytotoxic CD8+ T cells and IL-2 promoting the natural response of the organism to inflammation) [10,15]. There was no negative effect of the supplementation with Fe glycine chelate on the physical, morphometric, and strength parameters of tibiae, although the best results were obtained in groups receiving 40 mg and 10 mg Fe/kg of feed [16]. We also reported that the Fe glycine chelate supplementation of feed rations for Ross 308 broiler chickens had no negative effect on the chemical composition (fat, ash crude, protein, total cholesterol, total fatty acids: saturated fatty acids (SFAs), monounsaturated fatty acids (MUFAs), PUFAs, and unsaturated fatty acids (UFAs), and the n − 3/n − 6 fatty acid ratio) and on the sensory quality of thigh muscle [17]. In turn, in another study, we showed that Fe glycine chelate supplementation covering 50% and 25% of the demand (20 and 10 mg Fe/kg of feed, respectively) reduced the antioxidant stability of the thigh muscle of Ross 308 chickens, compared to the control group, which was manifested by an increase in malondialdehyde (MDA) levels [18].
2.2. Chickens and the Design of the Experiment
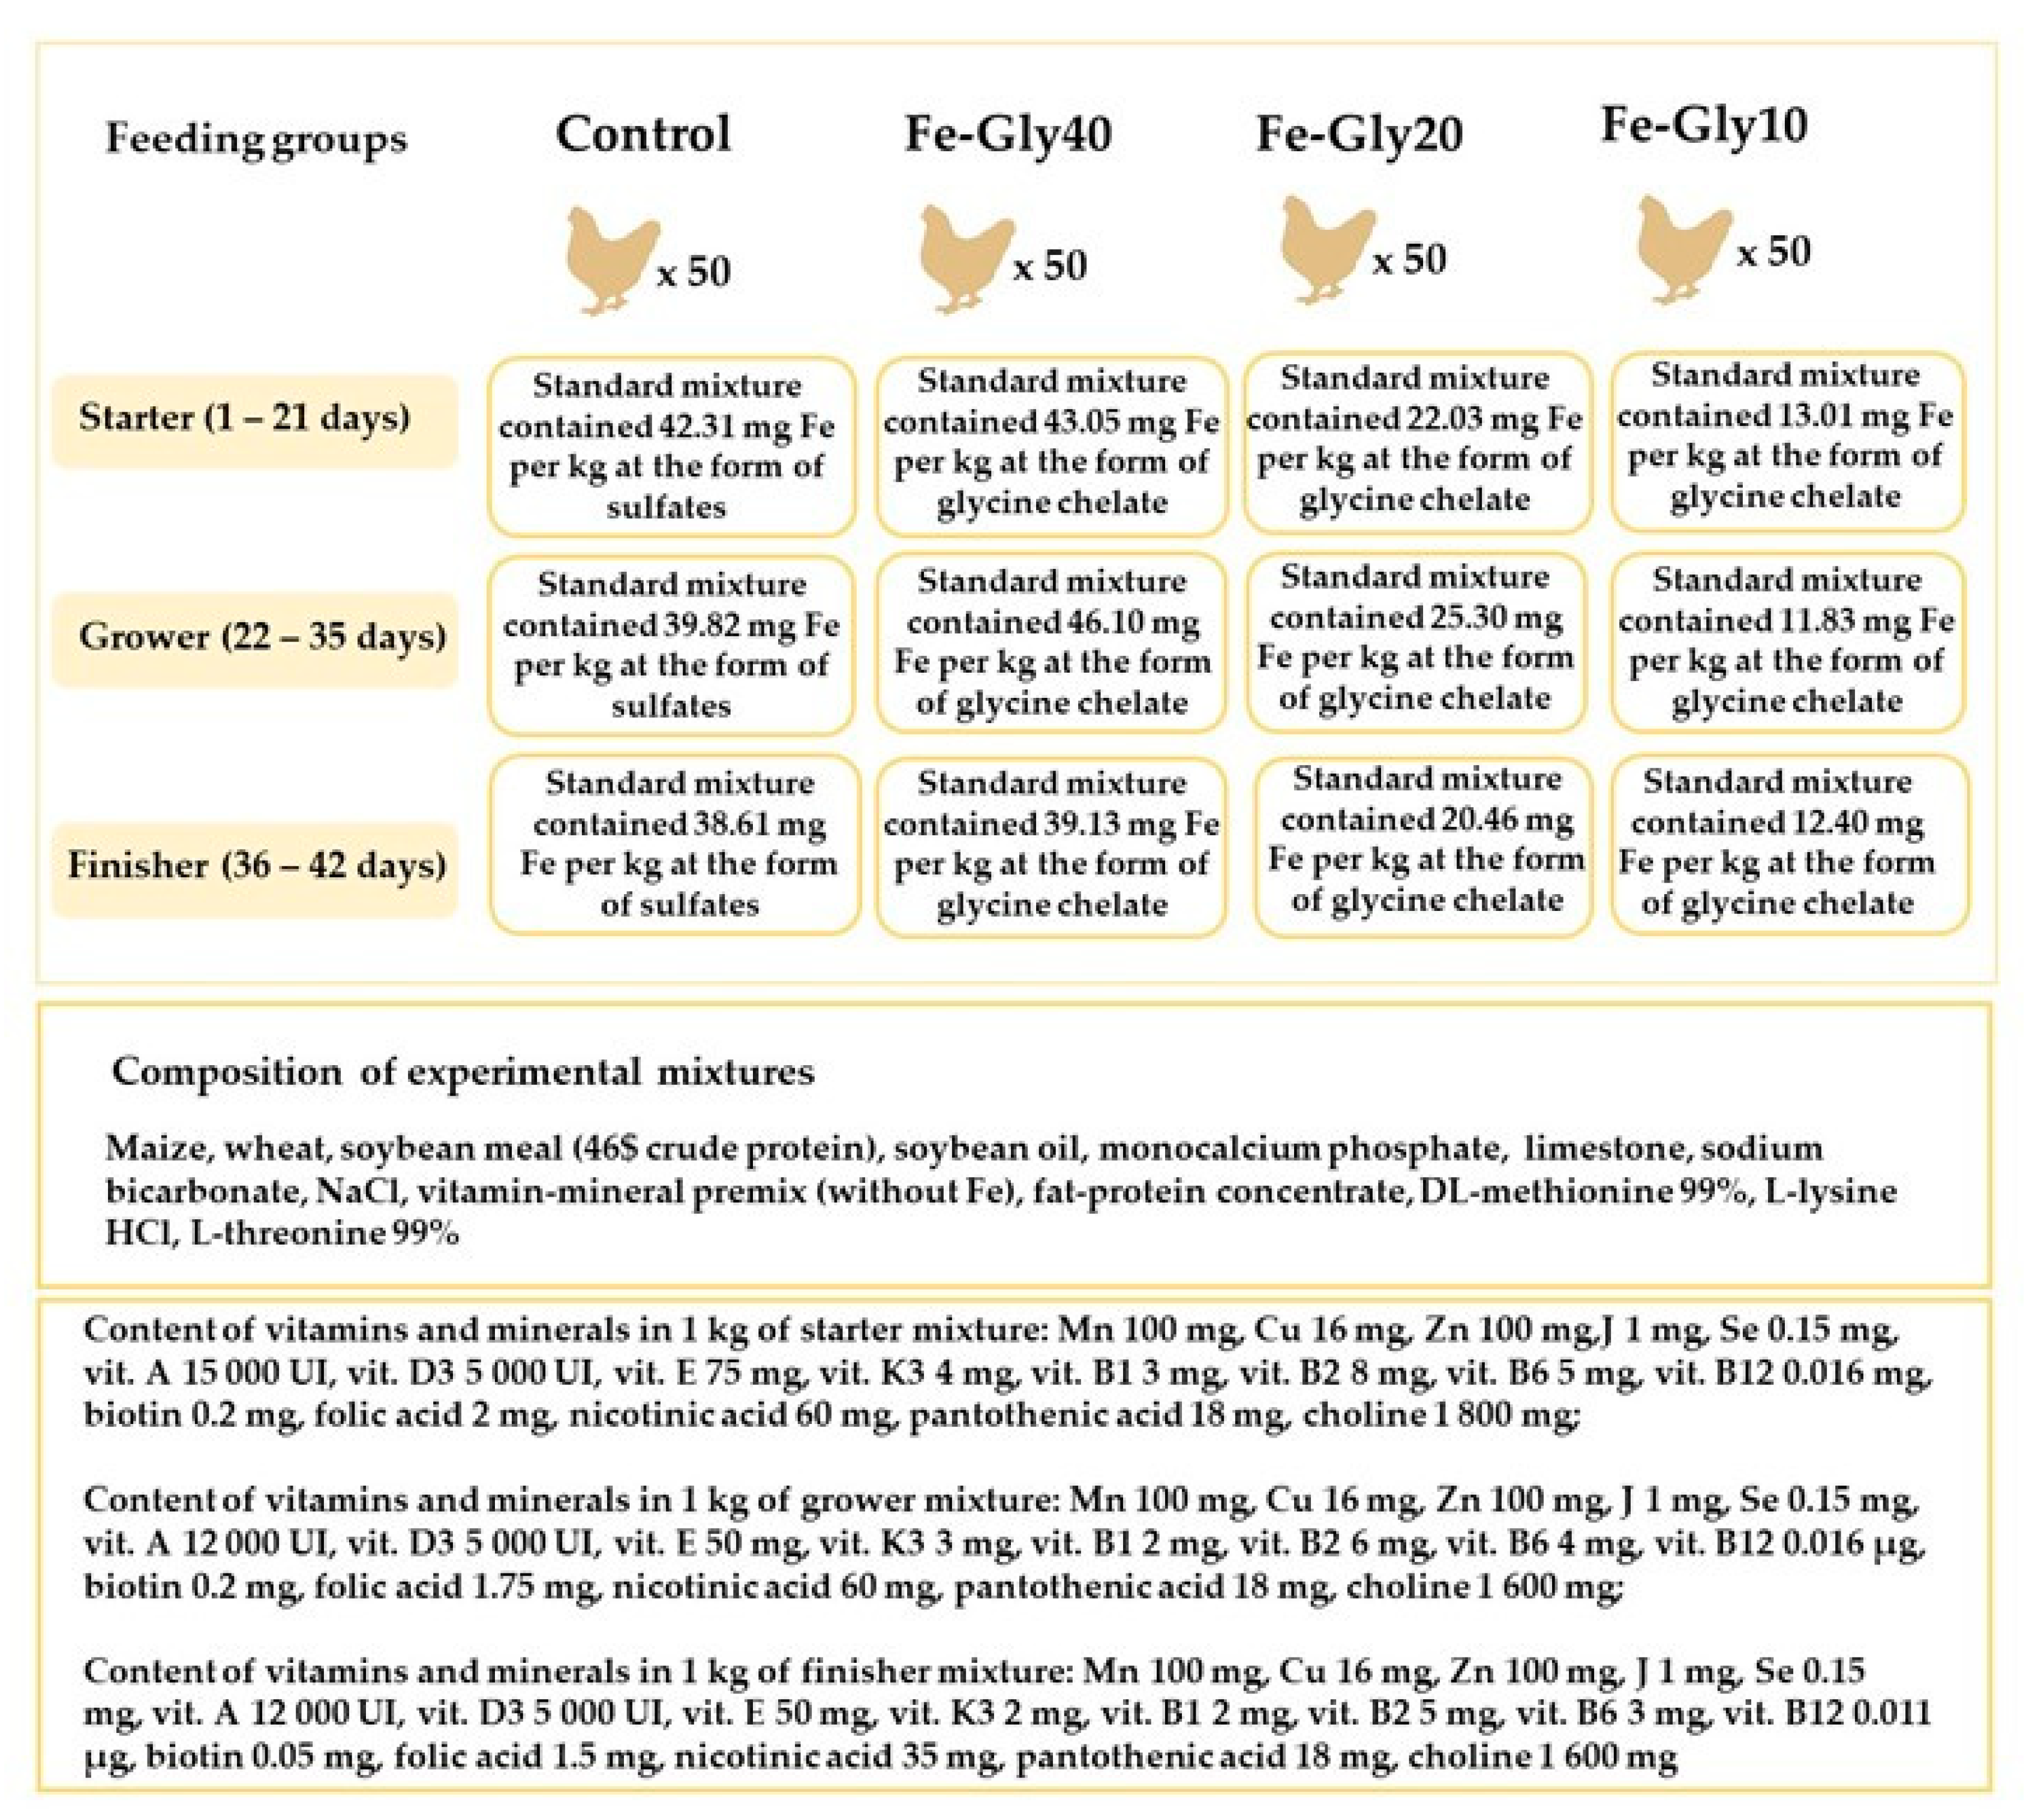
The 42-day investigations involved 200 chickens assigned into four dietary groups: the control receiving Fe sulfate in the dose of 40 mg/kg of feed and three experimental groups of chickens supplemented with 40 mg (Fe week until it reached 24°C -Gly40), 20 mg (Fe-Gly20), or 10 mg (Fe-Gly10) of Fe glycine chelate per 1 kg of feed (Figure 1). The initial temperature of 32°C was lowered by 2°C each [19]. The Fe demand was determined following the recommendations from Ross 308 chicken producers [20], while the feed mixtures supplied throughout the rearing stages (starter 1–21 days of age; grower 22–35 days of age; finisher 36–42 days of age) were optimized in accordance with the National Research Council (NRC) standards [21]. The nutritional value of the experimental mixtures is shown in Table 1, while Table 2 presents the FA profile in the basal feed mixture.
Figure 1.
Experimental design.
Table 1.
Nutritional value of experimental mixtures.
Table 2.
Fatty acids in basal mixtures in g/100g of total FA content.
2.3. Muscle Samples
The chickens were slaughtered on experimental day 42. The carcasses were cooled for 24 h at 4 °C and whole breast muscles were dissected, skinned, and transferred individually into resealable plastic bags, which were then kept in a freezer at −20 °C until chemical analyses [7].
2.4. Chemical Analyses
Prior to the chemical analyses, the meat was thawed at room temperature. The content of basic chemical components in the muscles and feed was determined using the AOAC method [22]: crude protein content with the Kjeldahl method, crude fat content with the Soxhlet method (SER 148 instrument from Velp, Italy), and crude ash content with the method of incineration in a muffle furnace (550 °C, oxidanthydrogen peroxide). The moisture content in the muscles was determined by drying the samples at 65 °C for 24 h. The Fe content in the incinerated samples was determined using the AAS method (Unicam 939 apparatus from AA Spectrometer Unicam; standards from Merck, Germany). The total cholesterol content was determined with the colorimetric method (EPOLL 20 colorimeter, from POLL Ltd., Warsaw, Poland; standard C3045 from Sigma, Ronkonkoma, NY, USA). The fatty acid profile was determined with the gas chromatography technique (Varian 3800 GC apparatus from Varian, The Netherlands) with an FID detector and a CP-Wax 52CBWCOT fused silica capillary column (60 min, internal diameter 0.25 mm, Supelco 37 standards FAME Mix 47885-U, Sigma, Poznań, Poland). The methods for the determination of the analyzed components were described in detail in our previous papers [6]. All chemical analyses were performed in triplicate.
2.5. Measurement of Meat pH
Meat pH was determined 15 and 45 min post slaughter as in Santé and Fernandez [23] (Testo 205 pH-meter from Testo AG, Titisee-Neustadt, Germany). The apparatus was calibrated with certified buffer solutions with pH 4.01 and 7.0. The same muscle sample was measured three times, and the mean pH value was calculated.
2.6. Calculations and Statistical Analysis
Based on the fatty acid content, Ʃ SFA, Ʃ MUFA, Ʃ PUFA, Ʃ UFA, Ʃ PUFA n − 3, Ʃ PUFA n − 6, Ʃ PUFA/SFA, Ʃ SFA/UFA, and the n − 6/n − 3 ratio were calculated.
Formulas developed by De Sousa et al. [24] were used to calculate the atherogenic index (AI), the thrombogenic index (TI), and the hypocholesterolemic/hypercholesterolemic (H/H) fatty acid ratio.
The results were analyzed statistically in the Statistica 6.0 program. Statistically significant differences (p < 0.05) in the mean values between the experimental groups were calculated with a one-way analysis of variance (ANOVA), the t-Student-Newman-Keuls test, and Tukey’s post hoc test.
3. Results
3.1. Content of Basic Chemical Components, Total Cholesterol Content, and pH
Table 3 shows data on the pH and chemical composition of the meat. The application of the different FeGly levels did not exert a statistically significant effect on the moisture level or the content of crude protein and total cholesterol in the breast muscle. Similarly, the pH value did not depend on the experimental factor. The crude ash content can be represented as Fe-Gly10 > Fe-Gly20 > Fe-Gly40 = control (p = 0.002). In turn, the crude fat content can be represented as Fe-Gly20 = Fe-Gly10 > Fe-Gly40, while the total fat content in the control group was not statistically different from the results obtained in the experimental groups (p = 0.02).
Table 3.
pH, moisture, and chemical composition of crude broiler breast meat.
3.2. Fatty Acid Profile in Breast Meat
Table 4 shows data on the FA profile in the meat. The Fe-Gly supplementation did not have a significant effect on the sum of SFAs, MUFAs, PUFAs, and UFAs in the breast muscle. However, the groups differed significantly in their content of individual fatty acids. The breast muscle in the Fe-Gly20 and Fe-Gly10 groups contained a significantly lower amount of myristic acid (C14:0) than that in the control. The breast muscle from these groups had a significantly higher content of eicosenoic acid (20:1n − 11) than the samples from the Fe-Gly40 group and significantly lower (p = 0.01) amounts of α-linoleic acid (18:3n − 3) than in the Fe-Gly40 and control groups.
Table 4.
Fatty acid profile (g/100 g of total FA) in broiler breast muscle.
3.3. Nutritional Value of Meat
The indices of the nutritional value of the meat are provided in Table 5. The experimental factor had no effect on the S/P indices (ratio of saturated to unsaturated fatty acids), the n − 6/n − 3 ratio, the TI value, and the H/H ratio. The level of Fe-Gly exerted a significant effect only on the AI value, which was significantly higher in the Fe-Gly20 and Fe-Gly10 groups than in the control. There was no difference in the AI value between the control and Fe-Gly40 groups and among the Fe-Gly40, Fe-Gly20, and Fe-Gly10 groups.
Table 5.
Indices of the nutritional value of meat.
4. Discussion
The present study showed no effect of the application of Fe glycine chelate on the content of crude protein in the chicken breast muscle, which proves that, despite its high biological importance, Fe even in the highly assimilable form does not substantially regulate protein synthesis in the organism, i.e., it does not increase muscle mass. These results are in agreement with our previous studies, where Fe glycine chelate supplementation had no impact on body weight gains and on the percentage proportion of breast and thigh muscles in carcasses [25]. Replacement of Fe sulfate with glycine chelate providing 40, 20, or 10 mg Fe/kg of feed reduced the content of fat in thigh muscle but had no effect on the protein content [17]. The content of crude fat in the breast muscle was significantly lower in the group receiving 40 mg Fe-Gly than in the group supplemented with 20 or 10 mg Fe-Gly, which confirms that higher levels of Fe in the organism inhibit lipogenesis.
Fe and lipid (including cholesterol) pathways change in response to changes in Fe levels in the organism [13]. Ferritin, i.e., an iron-storage protein modulating Fe uptake and release, is probably involved in these processes through inhibition of oxidative damage, lipid peroxidation, and various pro-inflammatory processes accompanying cellular stress [26]. Moreover, Fe is an integral part of some enzymes and transporters involved in lipid metabolism [27]. Fe has an impact on fat metabolism through the relationship between Fe metabolism and the amount of adipose tissue in the organism [28]. This is evidenced by the observation that a low level of Fe in the blood of obese subjects is probably caused by the impact of pro-inflammatory cytokines (chronic inflammation in obesity), i.e., strong inducers of the production of hepcidin in the liver, which inhibits ferroportin, thus reducing serum Fe levels and Fe availability in erythropoiesis [29]. As demonstrated in studies conducted on rats receiving a high-iron diet, Fe overload can impair lipid metabolism and reduce the expression of adiponectin and leptin [30,31]. The components of the Fe and erythropoiesis pathways modulate adipose tissue accumulation and glucose and lipid (including cholesterol) homeostasis [31].
As suggested by Ogłuszka et al. [32], there is a relationship between the level of n − 3 fatty acids and Fe metabolism; however, the mechanisms of the interaction have not been elucidated to date. A relationship between the Fe pathway and the synthesis and regulation of fatty acid levels has been observed e.g., in cancer cells [33]. Analyses of rats receiving high doses of Fe conducted by Valenzuela et al. [34] revealed reduced activity of Δ5 and Δ6 desaturases, i.e., key enzymes involved in the synthesis of long-chain n − 6 and n − 3 FAs. It resulted in a decrease in the PUFA level in the liver. In contrast, the present study showed no such effects. The supplementation with Fe glycine chelates had only a slight effect on the FA profile in the broiler breast muscle. Similarly, in our previous publication, we did not find a significant effect of Fe glycine chelate (10, 20, or 40 mg/kg of feed) on the sum of SFAs, MUFAs, and PUFAs and on the n − 6/n − 3 ratio in thigh muscles although there were differences in the content of some acids between the experimental groups [17]. The present analyses revealed that the Fe application did not have a significant effect on the content of arachidonic acid. As shown by research, enhanced release of arachidonic acid and eicosanoid compounds in iron-overloaded cardiomyocytes causes incorporation of this fatty acid into phosphatidylcholine as well as induction of cyclooxygenase-2 and production of eicosanoids [35]. Therefore, our results may indicate that the amount of Fe administered to chickens was not excessive.
The proportions between SFAs and UFAs as well as the levels of aldehydes, ketones, and alcohols determine the odor of meat, i.e., one of the most important organoleptic traits [17]. Since PUFAs are very sensitive to peroxidation leading to the formation of volatile and non-volatile compounds with an unpleasant odor, their content in meat is extremely important [36]. As shown in our previous study, in comparison with the control group, the Fe chelate supplementation was found to reduce the antioxidant stability in the thigh muscle, which lowered the quality of the meat [18] but did not have a significant effect on its sensory traits [17]. Noteworthy is the fact that mineral chelates used as supplementation of poultry feed are 2- or 3-fold more expensive than sulfates in Poland, but they are concurrently more readily assimilable [19].
The Ʃ PUFA-to-Ʃ SFA ratio in meat should be higher than 0.45, as lower values are responsible for a hypercholesterolemic effect on the human organism [37]. The Ʃ PUFA/Ʃ SFA proportion in all the groups analyzed in this study exceeded 0.88, i.e., the breast muscle had high anticholesterolemic potential. The content and ratio of n − 6 and n − 3 PUFAs determine the hypocholesterolemic index value, as n − 3 fatty acids play the main role in the regulation of the thrombogenic index and n − 6 fatty acids modulate the atherogenic index [38]. Meat with high dietary values is characterized by low AI and TI indices (1.0 and 0.5, respectively) and a high H/H index [19,38]. In the present study, the AI index in the chicken breast muscle was very low, i.e., slightly above 0.5. Noteworthy, the TI value in the experimental groups ranged from 1.02 (Fe-Gly40) to 1.08 (Fe-Gly10), i.e., it was approximately 50% higher than the recommended value. Nevertheless, we believe that one parameter that does not meet the recommendations should not have an impact on the general assessment of the dietary value of breast muscle from chickens supplemented with Fe glycine chelates. Noteworthy, the TI value in the control group was high as well, i.e., 1.06. The H/H ratio indicates that fatty acids have an effect on cholesterol metabolism; hence, the values of this parameter should be high [38]. In the present study, the H/H value in the experimental groups was in the range from 2.7 (Fe-Gly20) to approx. 2.8 (Fe-Gly40), while the ratio in the control group was below 0.6, i.e., it was approx. 80% lower than in the Fe-Gly supplemented groups.
5. Conclusions
To sum up, there was no negative effect of the supplementation of the nutrition for broiler chickens with Fe glycine chelate in amounts covering the demand in 100% (40 mg Fe/kg of feed) and at deficient levels covering the demand in 50% (20 mg Fe/kg of feed) and 25% (10 mg Fe/kg of feed) on the chemical composition and dietary quality of chicken breast muscle. The present results did not confirm a positive effect of these chelates on meat quality. Therefore, the use of Fe glycine chelates in the nutrition of broiler chickens should be reconsidered.
Author Contributions
Conceptualization, A.W.-M. and M.K.; methodology, A.W.-M. and M.K.; validation, A.W.-M., Z.Z. and D.Y.; formal analysis, K.J.-R., S.K. and Z.Z.; investigation, K.J.-R.; resources, M.K. and S.K.; data curation, A.W.-M.; writing—original draft preparation, A.W.-M.; writing—review and editing, M.K.; visualization, K.J.-R.; supervision, A.W.-M.; project administration, M.K.; funding acquisition, M.K. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by project NN 311543540 of the Ministry of Science and Higher Education, Poland.
Institutional Review Board Statement
The study was conducted according to the guidelines of the Declaration of Helsinki, and all the experimental procedures complied with the authorisation of the Local Ethics Committee for Animal Testing at the University of Natural Sciences in Lublin, Poland (Resolution No. 37/2011 of 17 May 2011).
Data Availability Statement
The data presented in this study are available on request from the corresponding author.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Dinh, T.T.N.; Thompson, L.D.; Galyean, M.L.; Brooks, J.C.; Patterson, K.Y.; Boylan, L.M. Cholesterol content and methods for cholesterol determination in meat and poultry. Compr. Rev. Food Sci. Food Saf. 2011, 10, 269–289. [Google Scholar] [CrossRef] [Scilit]
- Goluch, Z.; Słupczyńska, M.; Okruszek, A.; Haraf, G.; Wereńska, M.; Wołoszyn, J. The Energy and Nutritional Value of Meat of Broiler Chickens Fed with Various Addition of Wheat Germ Expeller. Animals 2023, 13, 499. [Google Scholar] [CrossRef] [Scilit]
- Pisulewski, P.M. Nutritional potential for improving meat quality in poultry. Anim. Sci. Pap. Rep. 2005, 23, 303–315. [Google Scholar]
- Long, S.; Liu, S.; Wu, D.; Mahfuz, S.; Piao, X. Effects of Dietary Fatty Acids from Different Sources on Growth Performance, Meat Quality, Muscle Fatty Acid Deposition, and Antioxidant Capacity in Broilers. Animals 2020, 10, 508. [Google Scholar] [CrossRef] [Scilit]
- Jachimowicz, K.; Winiarska-Mieczan, A.; Tomaszewska, E. The Impact of Herbal Additives for Poultry Feed on the Fatty Acid Profile of Meat. Animals 2022, 12, 1054. [Google Scholar] [CrossRef] [Scilit]
- Winiarska-Mieczan, A.; Kwiecień, M. The effects of copper-glycine complexes on chemical composition and sensory attributes of raw, cooked and grilled chicken meat. J. Food Sci. Tech. 2015, 52, 4226–4235. [Google Scholar] [CrossRef] [Scilit]
- Winiarska-Mieczan, A.; Kwiecień, M.; Kwiatkowska, K.; Baranowska-Wójcik, E.; Szwajgier, D.; Zaricka, E. Fatty acid profile, antioxidative status and dietary value of the breast muscle of broiler chickens receiving glycine-Zn chelates. Anim. Prod. Sci. 2020, 60, 1095–1102. [Google Scholar] [CrossRef] [Scilit]
- Zając, M.; Kiczorowska, B.; Samolińska, W.; Klebaniuk, R.; Andrejko, D.; Kiczorowski, P.; Milewski, S.; Winiarska-Mieczan, A. Supplementation of Broiler Chicken Feed Mixtures with Micronised Oilseeds and the Effects on Nutrient Contents and Mineral Profiles of Meat and Some Organs, Carcass Composition Parameters, and Health Status. Animals 2022, 12, 1623. [Google Scholar] [CrossRef] [Scilit]
- Lin, X.; Gou, Z.; Wang, Y.; Li, L.; Fan, Q.; Ding, F.; Zheng, C.; Jiang, S. Effects of Dietary Iron Level on Growth Performance, Immune Organ Indices and Meat Quality in Chinese Yellow Broilers. Animals 2020, 10, 670. [Google Scholar] [CrossRef] [Scilit]
- Jarosz, Ł.; Kwiecień, M.; Marek, A.; Grądzki, Z.; Winiarska-Mieczan, A.; Kalinowski, M.; Laskowska, E. Effects of feed supplementation with glycine chelate and iron sulfate on selected parameters of cell-mediated immune response in broiler chickens. Res. Vet. Sci. 2016, 107, 68–74. [Google Scholar] [CrossRef] [Scilit]
- Tang, L.; Zhang, Y.; Qian, Z.; Shen, X. The mechanism of Fe2+-initiated lipid peroxidation in liposomes: The dual function of ferrous ions, the roles of the pre-existing lipid peroxides and the lipid peroxyl radical. Biochem. J. 2000, 352, 27–36. [Google Scholar] [CrossRef]
- Kwiecień, M.; Winiarska-Mieczan, A.; Milczarek, A.; Klebaniuk, R. Biological response of broiler chickens to decreasing dietary inclusion levels of zinc glycine chelate. Biol. Trace Elem. Res. 2017, 175, 204–213. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rockfield, S.; Chhabra, R.; Robertson, M.; Rehman, N.; Bisht, R.; Nanjundan, M. Links between iron and lipids: Implications in some major human diseases. Pharmaceuticals 2018, 11, 113. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, M.; Chen, H.; Ailati, A.; Chen, W.; Chilton, F.H.; Lowther, W.T.; Chen, Y.Q. Substrate specificity and membrane topologies of the iron-containing ω3 and ω6 desaturases from Mortierella alpina. Appl. Microbiol. Biotechnol. 2018, 102, 211–223. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kwiecień, M.; Samolińska, W.; Bujanowicz-Haraś, B. Effects of iron-glycine chelate on growth, carcass characteristic, liver mineral concentrations and haematological and biochemical blood parameters in broilers. J. Anim. Physiol. Anim. Nutr. 2015, 99, 1184–1196. [Google Scholar] [CrossRef] [Scilit]
- Kwiatkowska, K.; Winiarska-Mieczan, A.; Kwiecień, M. Effect of application of Fe-glycinate chelate in diet for broiler chickens in an amount covering 50 or 25% of the requirement on physical, morphometric, and strength parameters of tibia bones. Biol. Trace Elem. Res. 2018, 184, 483–490. [Google Scholar] [CrossRef] [Scilit]
- Winiarska-Mieczan, A.; Kwiecień, M.; Grela, E.R.; Tomaszewska, E.; Klebaniuk, R. The chemical composition and sensory properties of raw, cooked and grilled thigh meat of broiler chickens fed with Fe-Gly chelate. J. Food Sci. Tech. 2016, 53, 3825–3833. [Google Scholar] [CrossRef] [Scilit]
- Winiarska-Mieczan, A.; Kwiecień, M.; Mieczan, T.; Kwiatkowska, K.; Jachimowicz, K. The effect of Cu, Zn and Fe chelates on the antioxidative status of thigh meat of broiler chickens. Animal 2021, 15, 100367. [Google Scholar] [CrossRef] [Scilit]
- Winiarska-Mieczan, A.; Jachimowicz, K.; Kwiecień, M.; Kislova, S.; Baranowska-Wójcik, E.; Zasadna, Z.; Yanovych, D.; Kowalczuk-Vasilev, E. The Impact of Zn, Cu and Fe Chelates on the Fatty-Acid Profile and Dietary Value of Broiler-Chicken Thigh Meat. Animals 2021, 11, 3115. [Google Scholar] [CrossRef] [Scilit]
- Aviagen. Ross 308 Parent Stock: Nutrition Specifications. Available online: www.aviagen.com (accessed on 20 October 2019).
- NRC. National Research Council. Nutrient Requirements of Poultry; National Academy Press: Washington, DC, USA, 1994. [Google Scholar]
- AOAC. Official Methods of Analysis, 17th ed.; AOAC International: Gaithersburg, MA, USA, 2000. [Google Scholar]
- Santé, V.; Fernandez, X. The measurement of pH in raw and frozen turkey Pectoralis superficial is muscle. Meat Sci. 2000, 55, 503–506. [Google Scholar] [CrossRef] [Scilit]
- De Sousa, A.B.B.; de Santos Júnior, O.; Visentainer, J.V.; de Almeida, N.M. Total lipid nutritional quality of the adipose tissue from the orbital cavity in Nile tilapia from continental aquaculture. Acta Sci. Anim. Sci. 2017, 39, 335–341. [Google Scholar] [CrossRef] [Scilit]
- Kwiecień, M.; Winiarska-Mieczan, A.; Milczarek, A.; Tomaszewska, E.; Matras, J. Effects of zinc glycine chelate on growth performance, carcass characteristics, bone quality, and mineral content in bone of broiler chicken. Livest. Sci. 2016, 191, 43–50. [Google Scholar] [CrossRef] [Scilit]
- Bu, W.; Liu, R.; Cheung-Lau, J.C.; Dmochowski, I.J.; Loll, P.J.; Eckenhoff, R.G. Ferritin couples iron and fatty acid metabolism. FASEB J. 2012, 26, 2394–2400. [Google Scholar] [CrossRef] [PubMed]
- Ahmed, U.; Latham, P.S.; Oates, P.S. Interactions between hepatic iron and lipid metabolism with possible relevance to steatohepatitis. World J. Gastroenterol. 2012, 18, 4651–4658. [Google Scholar] [CrossRef] [Scilit]
- Żekanowska, E.; Boinska, J.; Giemza-Kucharska, P.; Kwapisz, J. Obesity and iron metabolism. J. Biotech. Comput. Biol. Bionanotech. 2011, 92, 147–152. [Google Scholar] [CrossRef] [Scilit]
- Feldman, A.; Aigner, E.; Weghuber, D.; Paulmichl, K. The Potential Role of Iron and Copper in Pediatric Obesity and Nonalcoholic Fatty Liver Disease. Biomed. Res. Int. 2015, 2015, 287401. [Google Scholar] [CrossRef] [Scilit]
- Zhang, L.; Dai, X.; Wang, L.; Cai, J.; Shen, J.; Shen, Y.; Li, X.; Zhao, Y. Iron overload accelerated lipid metabolism disorder and liver injury in rats with non-alcoholic fatty liver disease. Front Nutr. 2022, 9, 961892. [Google Scholar] [CrossRef] [Scilit]
- Hilton, C.; Sabaratnam, R.; Drakesmith, H.; Karpe, F. Iron, glucose and fat metabolism and obesity: An intertwined relationship. Int. J. Obes. 2023, 47, 554–563. [Google Scholar] [CrossRef] [Scilit]
- Ogłuszka, M.; Lipiński, P.; Starzyński, R.R. Interaction between iron and omega-3 fatty acids metabolisms: Where is the cross-link? Crit. Rev. Food Sci. Nutr. 2022, 62, 3002–3022. [Google Scholar] [CrossRef] [Scilit]
- Konstorum, A.; Lynch, M.L.; Torti, S.V.; Torti, F.M.; Laubenbacher, R.C. A Systems Biology Approach to Understanding the Pathophysiology of High-Grade Serous Ovarian Cancer: Focus on Iron and Fatty Acid Metabolism. Omics A J. Integr. Biol. 2018, 22, 502–513. [Google Scholar] [CrossRef] [Scilit]
- Valenzuela, R.; Rincon-Cervera, M.A.; Echeverria, F.; Barrera, C.; Espinosa, A.; Hernandez-Rodas, M.C.; Ortiz, M.; Valenzuela, A.; Videla, L.A. Iron-induced pro-oxidant and pro-lipogenic responses in relation to impaired synthesis and accretion of long-chain polyunsaturated fatty acids in rat hepatic and extrahepatic tissues. Nutrition 2018, 45, 49–58. [Google Scholar] [CrossRef] [Scilit]
- Mattera, R.; Stone, G.P.; Bahhur, N.; Kuryshev, Y.A. Increased release of arachidonic acid and eicosanoids in iron-overloaded cardiomyocytes. Circulation 2001, 103, 2395–2401. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Łopacka, J.; Lipińska, A. Oxidative changes during storage of beef under modified atmosphere and thermal treatment and its potential impact on human health. Probl. Hig. Epidemiol. 2015, 96, 719–726. [Google Scholar]
- Mapiye, C.; Chimonyo, M.; Dzama, K.; Hugo, A. Fatty acid composition of beef from Nguni steers supplemented with Acacia karroo leaf-meal. J. Food Compos. Anal. 2011, 24, 523–528. [Google Scholar] [CrossRef] [Scilit]
- Woloszyn, M.R.; Clyde, K.; Corno, D. The relative impact of looks, income, warmth, and intelligence on female online dating preferences. Soc. Sci. Humanit. Open 2020, 2, 100089. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2023 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).