Article

Cultivar-Specific Expression of the Vintage Effect in Furmint Grapes from the Tokaj Wine Region; Part II: Acid Balance, Potassium Accumulation and Tannin Content


1
Centre for Precision Farming R&D Services, Faculty of Agricultural and Food Sciences and Environmental Management, University of Debrecen, H-4032 Debrecen, Hungary
2
Szepsy Winery, H-3909 Mád, Hungary
3
Research Laboratory and Wine Academy of Mad, University of Debrecen, H-3909 Mád, Hungary
*
Author to whom correspondence should be addressed.
Agronomy 2026, 16(13), 1253; https://doi.org/10.3390/agronomy16131253
Submission received: 30 May 2026 / Revised: 22 June 2026 / Accepted: 26 June 2026 / Published: 29 June 2026
(This article belongs to the Section Horticultural and Floricultural Crops)

Abstract

Understanding how interannual climatic variability shapes must composition is critical for predicting wine quality under warming conditions, particularly for acid-retaining cultivars such as Vitis vinifera L. cv. Furmint. This study—conducted as a continuation of a previous investigation on Furmint berry weight, total soluble solids and total dry extract—evaluated titratable acidity, pH, potassium, ammonia and tannin content across three contrasting vintages (2022–2024) in the Tokaj wine region. Using a high-resolution meteorological dataset and an extensive climatic parameter matrix, exploratory analysis was conducted to evaluate responses, and the most influential thermal, radiation-related and water-balance related climatic factors associated with each must parameter were identified. Total acidity and pH showed consistent sensitivity to climatic variability: acidity decreased with mid-season warm nights and abundant summer rainfall, while pH was inversely associated with extreme heat events but increased under higher early-season rainfall and post-véraison irradiation. Potassium content exhibited partly atypical responses, showing positive correlations with late-season warm nights and frequent summer precipitation, and negative with early heat. Ammonia displayed weak to moderate climatic dependence, while tannic acid consistently decreased with higher thermal and irradiation loads. Overall, these results imply cultivar-specific climatic responses in Furmint and suggest that temperature extremes, nighttime heat and rainfall timing are important factors shaping must composition, providing a foundation to better understand the expression of vintage effects under climate change.

1. Introduction

The composition of grape must—including titratable acidity, pH, mineral cations, yeast-assimilable nitrogen (YAN), and phenolic (tannin) content—is a primary determinant of future wine style, microbial stability, and aging potential. While the literature provides extensive evidence on how climate modulates sugar accumulation and polyphenol content, comparatively fewer studies have quantified how interannual climatic variability influences the broader suite of must quality attributes that determine wine stability, fermentation behavior, and sensory profile.
In our previous study on Furmint [1], we characterized vintage variation in berry weight, total soluble solids and total dry extract across three consecutive seasons in the Tokaj region; those results highlighted the importance of water availability and early phenological climate as descriptors of vintage effects. However, sugar-centered metrics alone are insufficient to predict wine composition and technological behavior under a warming climate as shifting thermal regimes increasingly decouple sugar accumulation from the evolution of other quality traits [2,3]. The present study builds directly on that earlier work, extending the analysis to a broader suite of must quality parameters that are critical for the chemical and technological stability of the must [4], while relying on the same vineyard network, sampling design and high-resolution meteorological dataset.
Titratable acidity and pH play fundamental roles in freshness, microbial stability, and wine balance. They are regulated by the concentrations of the major organic acids and by cation levels, most notably potassium (K). Potassium accumulates in berries during ripening and can neutralize tartaric acid, increasing must pH; warming and water stress have been associated with enhanced K+ accumulation and accelerated acid degradation [5,6].
Yeast-assimilable nitrogen—of which ammoniacal nitrogen represents a critical inorganic fraction—is essential for fermentation kinetics and aroma development, as it supports yeast metabolism. Low YAN levels may lead to sluggish or stuck fermentations and altered aroma profiles [7]. While present predominantly as the ammonium ion (NH4+) at typical grape must pH, this fraction is conventionally referred to as ammonia in enological contexts. Ammoniacal nitrogen levels exhibit strong dependence on grape variety and, importantly, are sensitive to climatic conditions [8].
Phenolic compounds, including tannins, influence mouthfeel, oxidative stability, and structural complexity. Their biosynthesis and extractability are responsive to temperature, radiation exposure, and water availability, though the magnitude and direction of these effects may vary by cultivar and terroir. Tannin content, particularly in late phenological phases, appears sensitive to drought stress—an increasingly frequent phenomenon in continental wine regions [9,10].
Collectively, the literature points to plausible mechanistic links between climatic drivers (temperature, radiation, precipitation, and water balance) and must acidity, pH, K+ concentration, YAN composition, and tannin levels. Nevertheless, significant knowledge gaps persist. Many studies focus on individual cultivars, single vineyards, or short time series; regionally specific data for Central-Eastern European continental terroirs such as Tokaj remain limited; and few analyses integrate high-resolution meteorological monitoring with extensive climatic-parameter matrices to predict these must components [11,12].
Therefore, this study extends our earlier work by analyzing titratable acidity, pH, potassium concentration, ammonia (as a proxy for YAN), and tannin content in Furmint musts sampled across the same vineyard network and the same three vintages (2022–2024). Building on the identical meteorological dataset and protocol used previously, this study aims to quantify vintage and environmental effects on this expanded set of must parameters, and to identify the specific climatic factors explaining their interannual variability. By evaluating how thermal conditions, precipitation patterns, and water balance shape the acidity, pH, potassium, nitrogen forms, and tannin accumulation of Furmint, we provide a direct assessment of this cultivar’s physiological and compositional responsiveness. Understanding these relationships is essential for adapting vineyard management to warming conditions, where preserving balanced acidity and overall typicity represents a critical challenge.

2. Materials and Methods

2.1. Study Area and Plant Material

This study was conducted in four vineyards of the Tokaj wine region (NE Hungary): Szent Tamás, Betsek, Kővágó, and Szilvás, all situated near Mád (N48.193127, E21.278096). These sites represent a compact but topographically diverse volcanic terroir, characterized by rhyolitic and zeolitic parent materials and clay-rich soils. Their slope exposure varies from south to east, whereas Szilvás is a nearly level valley-floor site.
Furmint was the sole cultivar examined. The vineyards are dominated by single-cordon-trained vines, mostly 20–30 years old, with the exception of Kővágó, replanted in 2017. Cultivation parameters were similar across the sites, featuring a row spacing of 2.2–2.8 m and a vine spacing of 0.7–1.1 m, which is typical for Furmint production in the Tokaj Wine Region. As is characteristic of long-established commercial production zones in this region, these vineyards feature mixed clonal material and traditional rootstocks; the microclimatic sampling network was specifically designed to capture the overarching vintage-driven responses across this heterogeneous production baseline, rather than isolating single-vine clonal or rootstock variables.
A more detailed account of the cultivar, terroir, site characteristics and soil descriptions is provided in our previous study focusing on berry growth and sugar accumulation. The experimental design and the microclimatic monitoring network were identical to those described in [1]. As this was a commercial, on-farm study conducted across production vineyards, routine pest management and maintenance fertilization were managed independently by the respective estates according to conventional regional practices. Because our primary objective is to isolate the dominant macro- and microclimatic drivers of the vintage effect, these localized agronomic variations represent secondary, non-climatic background variables and were not tracked individually.

2.2. Meteorological Monitoring

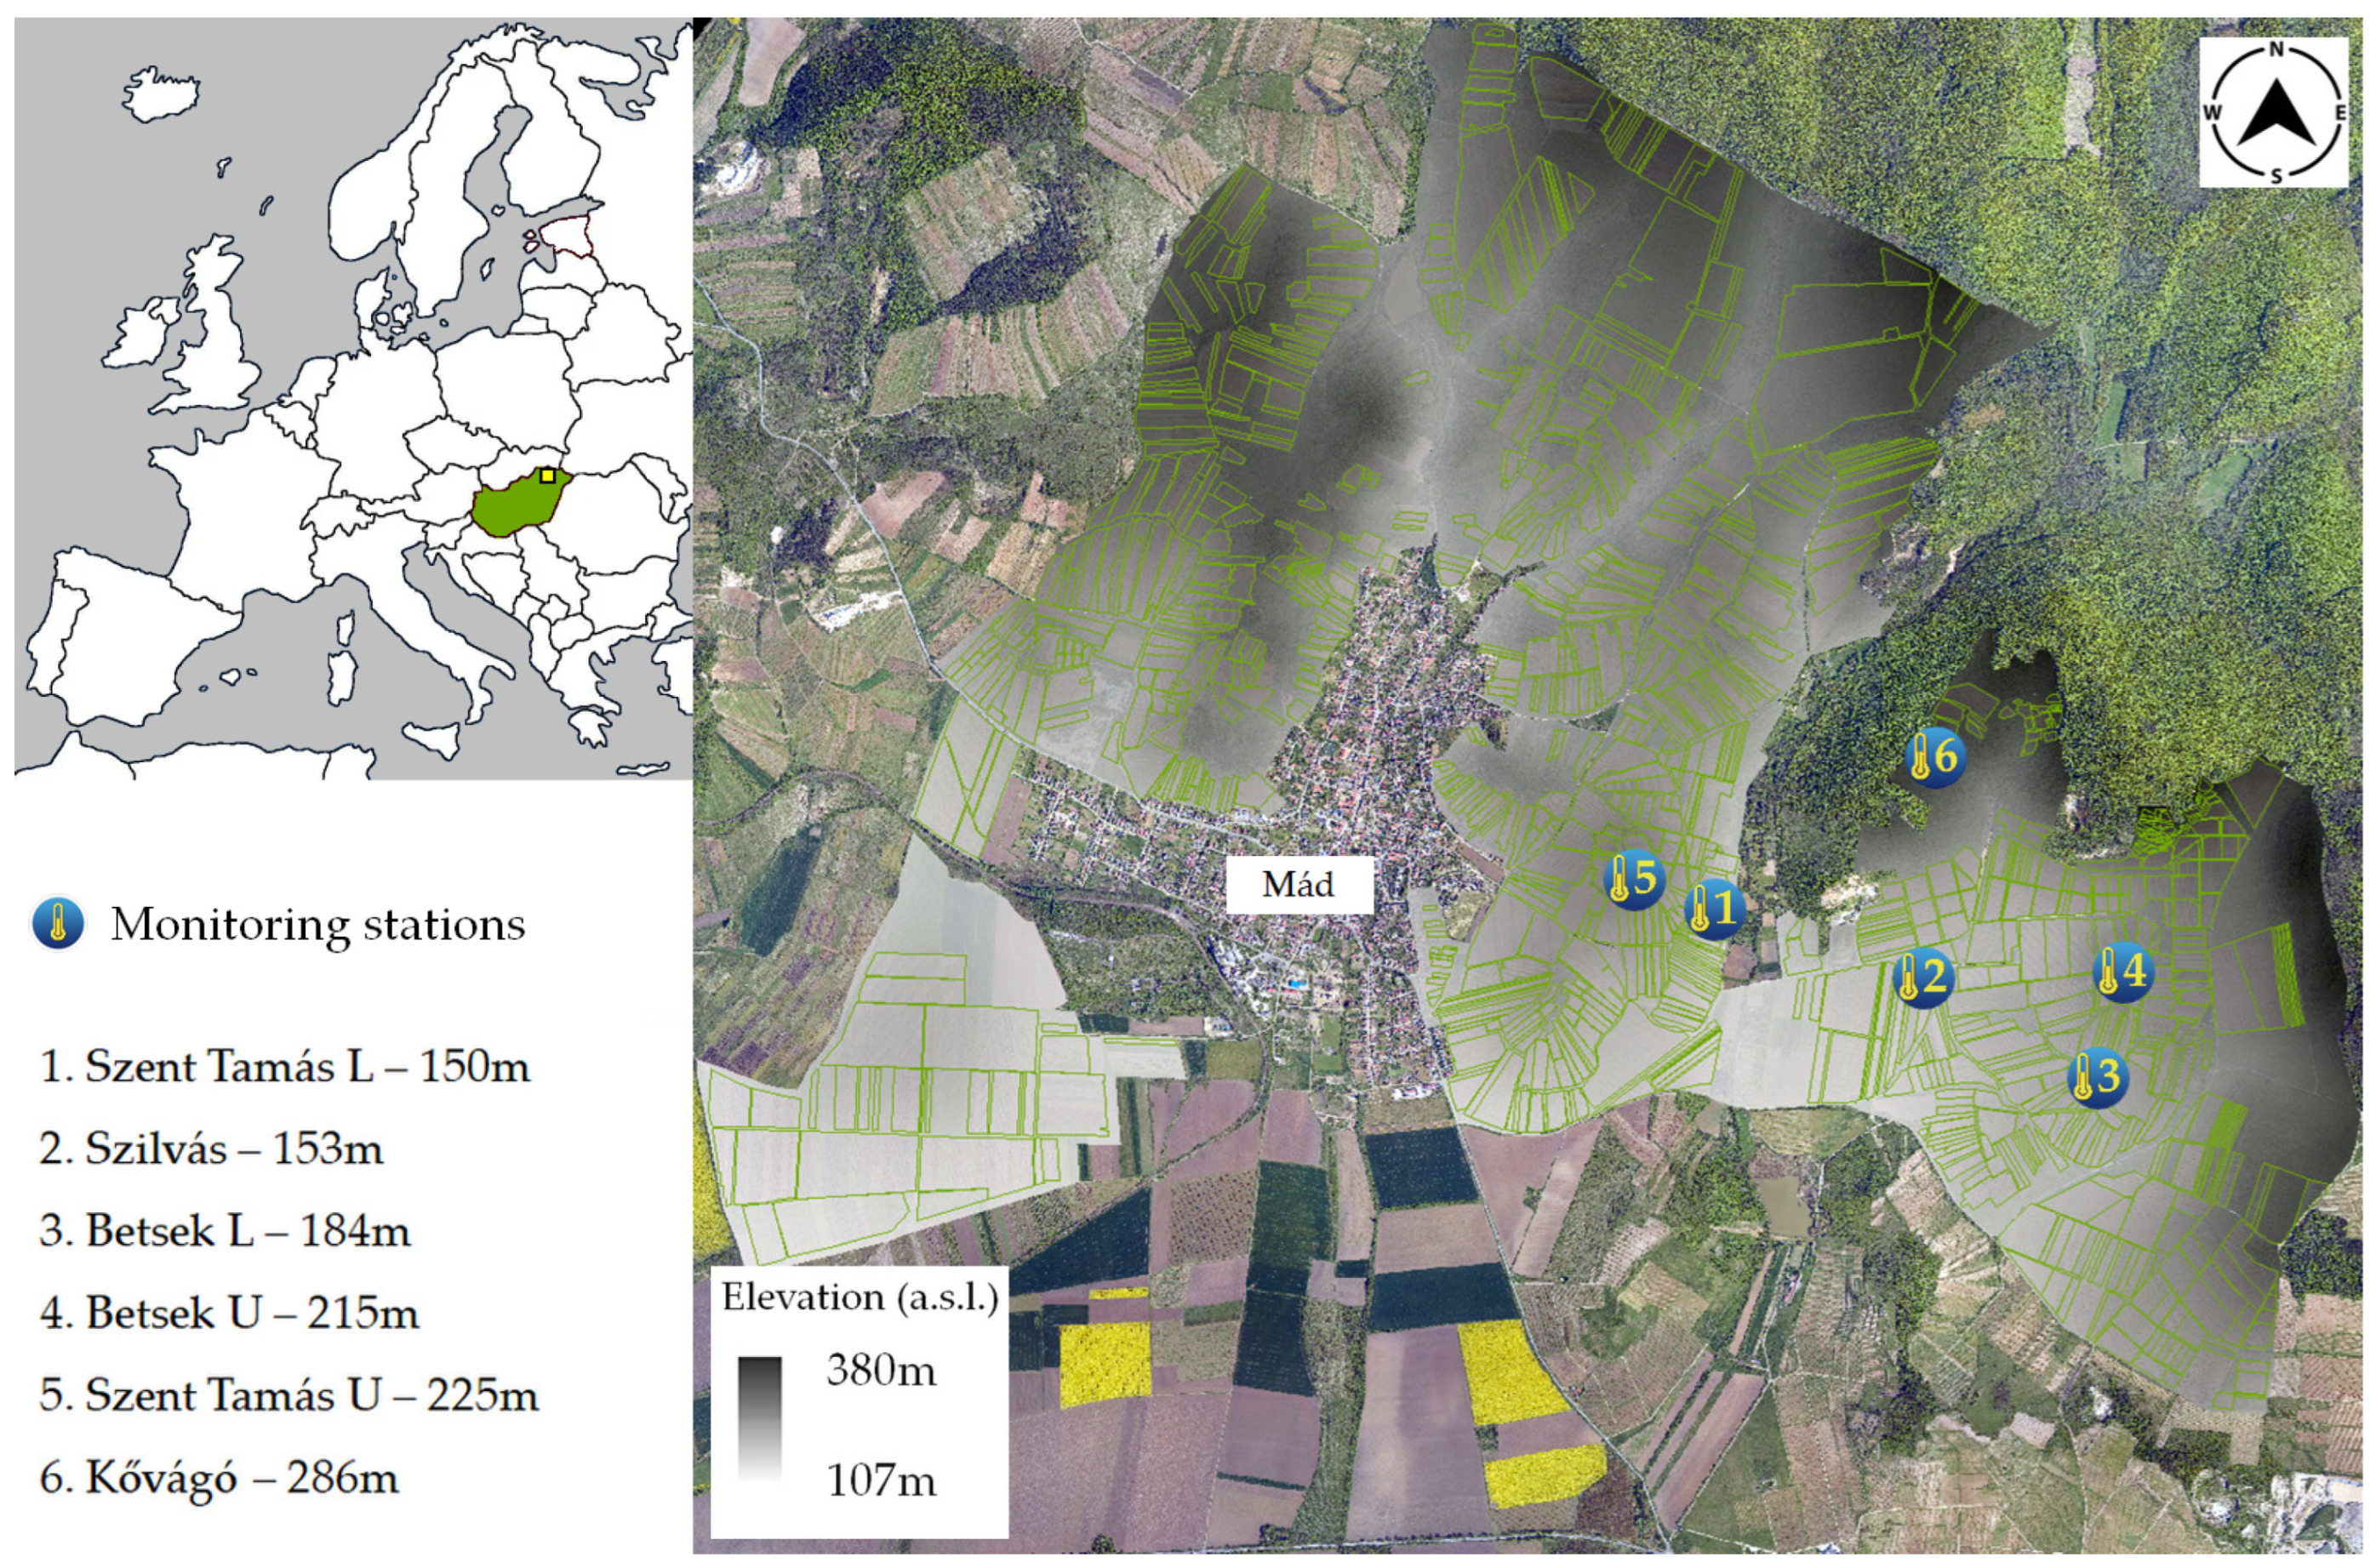
Six monitoring stations were positioned to capture the main topo-climatic contrasts of the study area, with three located on lower slopes or valley-bottom sites and three on upper slopes between 150 and 300 m a.s.l (Figure 1). The specific criteria for station siting prioritized: (i) representing the primary topographic and elevation gradients characteristic of the local terroir, and (ii) satisfying the World Meteorological Organization (WMO) exposure guidelines for agrometeorological observations, ensuring unimpeded solar radiation and wind exposure away from immediate canopy interference.
The sensors were installed at 2 m, positioned above the trellis system. The ClimaVue 50 sensors, connected to CR1000 dataloggers (Campbell Scientific, Logan, UT, USA), provided high-precision measurements, including air temperature (accuracy of ±0.6 °C), solar radiation (±5%), and precipitation (±5%). Data continuity was strictly monitored, with a data recovery rate exceeding 99% throughout the entire observation period. The measurements logged at 10 s frequency were aggregated to 10 min and, subsequently, daily values.
Phenology and vine sap flow were monitored throughout the 2022–2024 seasons using EXO-Skin SGEX-25 sensors (Dynamax Inc., Houston, TX, USA). The boundaries of the growing seasons were determined using a combined approach of thermal and physiological indicators calculated strictly on a site-specific basis for each individual monitoring location to capture topoclimatic variations. Sap flow intensity was utilized exclusively to pinpoint the physiological start (budburst) and the absolute end of vegetative activity. Budburst (the start of the growing season) was defined as the point when cumulative Growing Degree Days (GDD) reached 40 °C and sap flow intensity at least at two sensors out of three at that specific site exceeded 2% of its seasonal maximum. Conversely, the end of the season was identified when sap flow activity consistently dropped below this 2% threshold, marking the physiological transition to dormant stage.

2.3. Must Composition Analysis

To ensure maximum conformity with real-world wine production, the timing of sample collection was synchronized with the commercial harvesting practices of the local estates rather than applying artificial maturity thresholds. Harvest sampling followed a standardized protocol in which 200–250 berries were taken from 20 clusters of 5 vines at each site within a 10 m radius of each monitoring station to ensure spatial representativeness. Following transport (at +5 °C), fresh berry mass was measured using a precision balance (VWR TP2202, VWR International, Radnor, PA, USA), and berry juice was extracted using standardized centrifugation (MegaStar 1.6R centrifuge, VWR International, Lutterworth, UK) operated at 4500 rpm for 10 min.
Berry juice was analyzed for total acidity, pH, potassium (K+) and ammonium (NH4+) concentrations using Fourier-transform infrared spectroscopy (WineScan, Foss Electric, Hillerød, Denmark). Additionally, extractable tannin concentrations were quantified. While technically determined and calculated photometrically after extraction with dimethylformamide and reaction with iron (III)–ammonium citrate, measured at 525 nm (Lambda 25, PerkinElmer Inc., Waltham, MA, USA) as tannic acid equivalents (TAE) via spectrophotometry, this fraction is conventionally referred to as tannic acid or tannins throughout the manuscript. The analytical workflow largely parallels that described in our previous study, but here it is extended to include a wider suite of must parameters.

2.4. Data Processing and Statistical Evaluation

All must and climatic variables were processed in SPSS 28.0 (IBM Inc., Armonk, NY, USA). Derived climatic indices were computed in Microsoft Excel® for Microsoft 365 (version 2502).

2.5. Climatic Parameter Framework

2.5.1. Construction of the Parameter Matrix

To identify climate–must relationships, we assembled an extensive set of climatic descriptors, including classical viticultural indices, short phenology-based windows (instead of entire vintages), and multi-parameter combinations. Table A1 and Table A2 (Appendix A) provide the full list of variables used here.

2.5.2. Selection Procedure

Normality was tested using Kolmogorov–Smirnov and Shapiro–Wilk tests. Climate–must associations were quantified using Pearson or Spearman correlation, depending on distributional assumptions, and the 50 strongest correlates for each must variable were retained.
To ensure that only climate variables expressing genuine interannual variation were considered, vintage effects were tested by one-way ANOVA or the Kruskal–Wallis test. Parameters lacking significant vintage discrimination (p < 0.05) were removed. Subsequently, temporal relevance to grapevine physiology served as an exclusion criterion. When multiple variables covered similar intervals, preference was given to phenology-linked or shorter, more temporally focused descriptors.

2.5.3. Index Definitions

The complete set of bioclimatic parameters, along with their formal definitions, abbreviations, calculation methodologies, and standard references, is compiled in Table A3 (Appendix B).

3. Results

3.1. Climatic Context of the Three Vintages

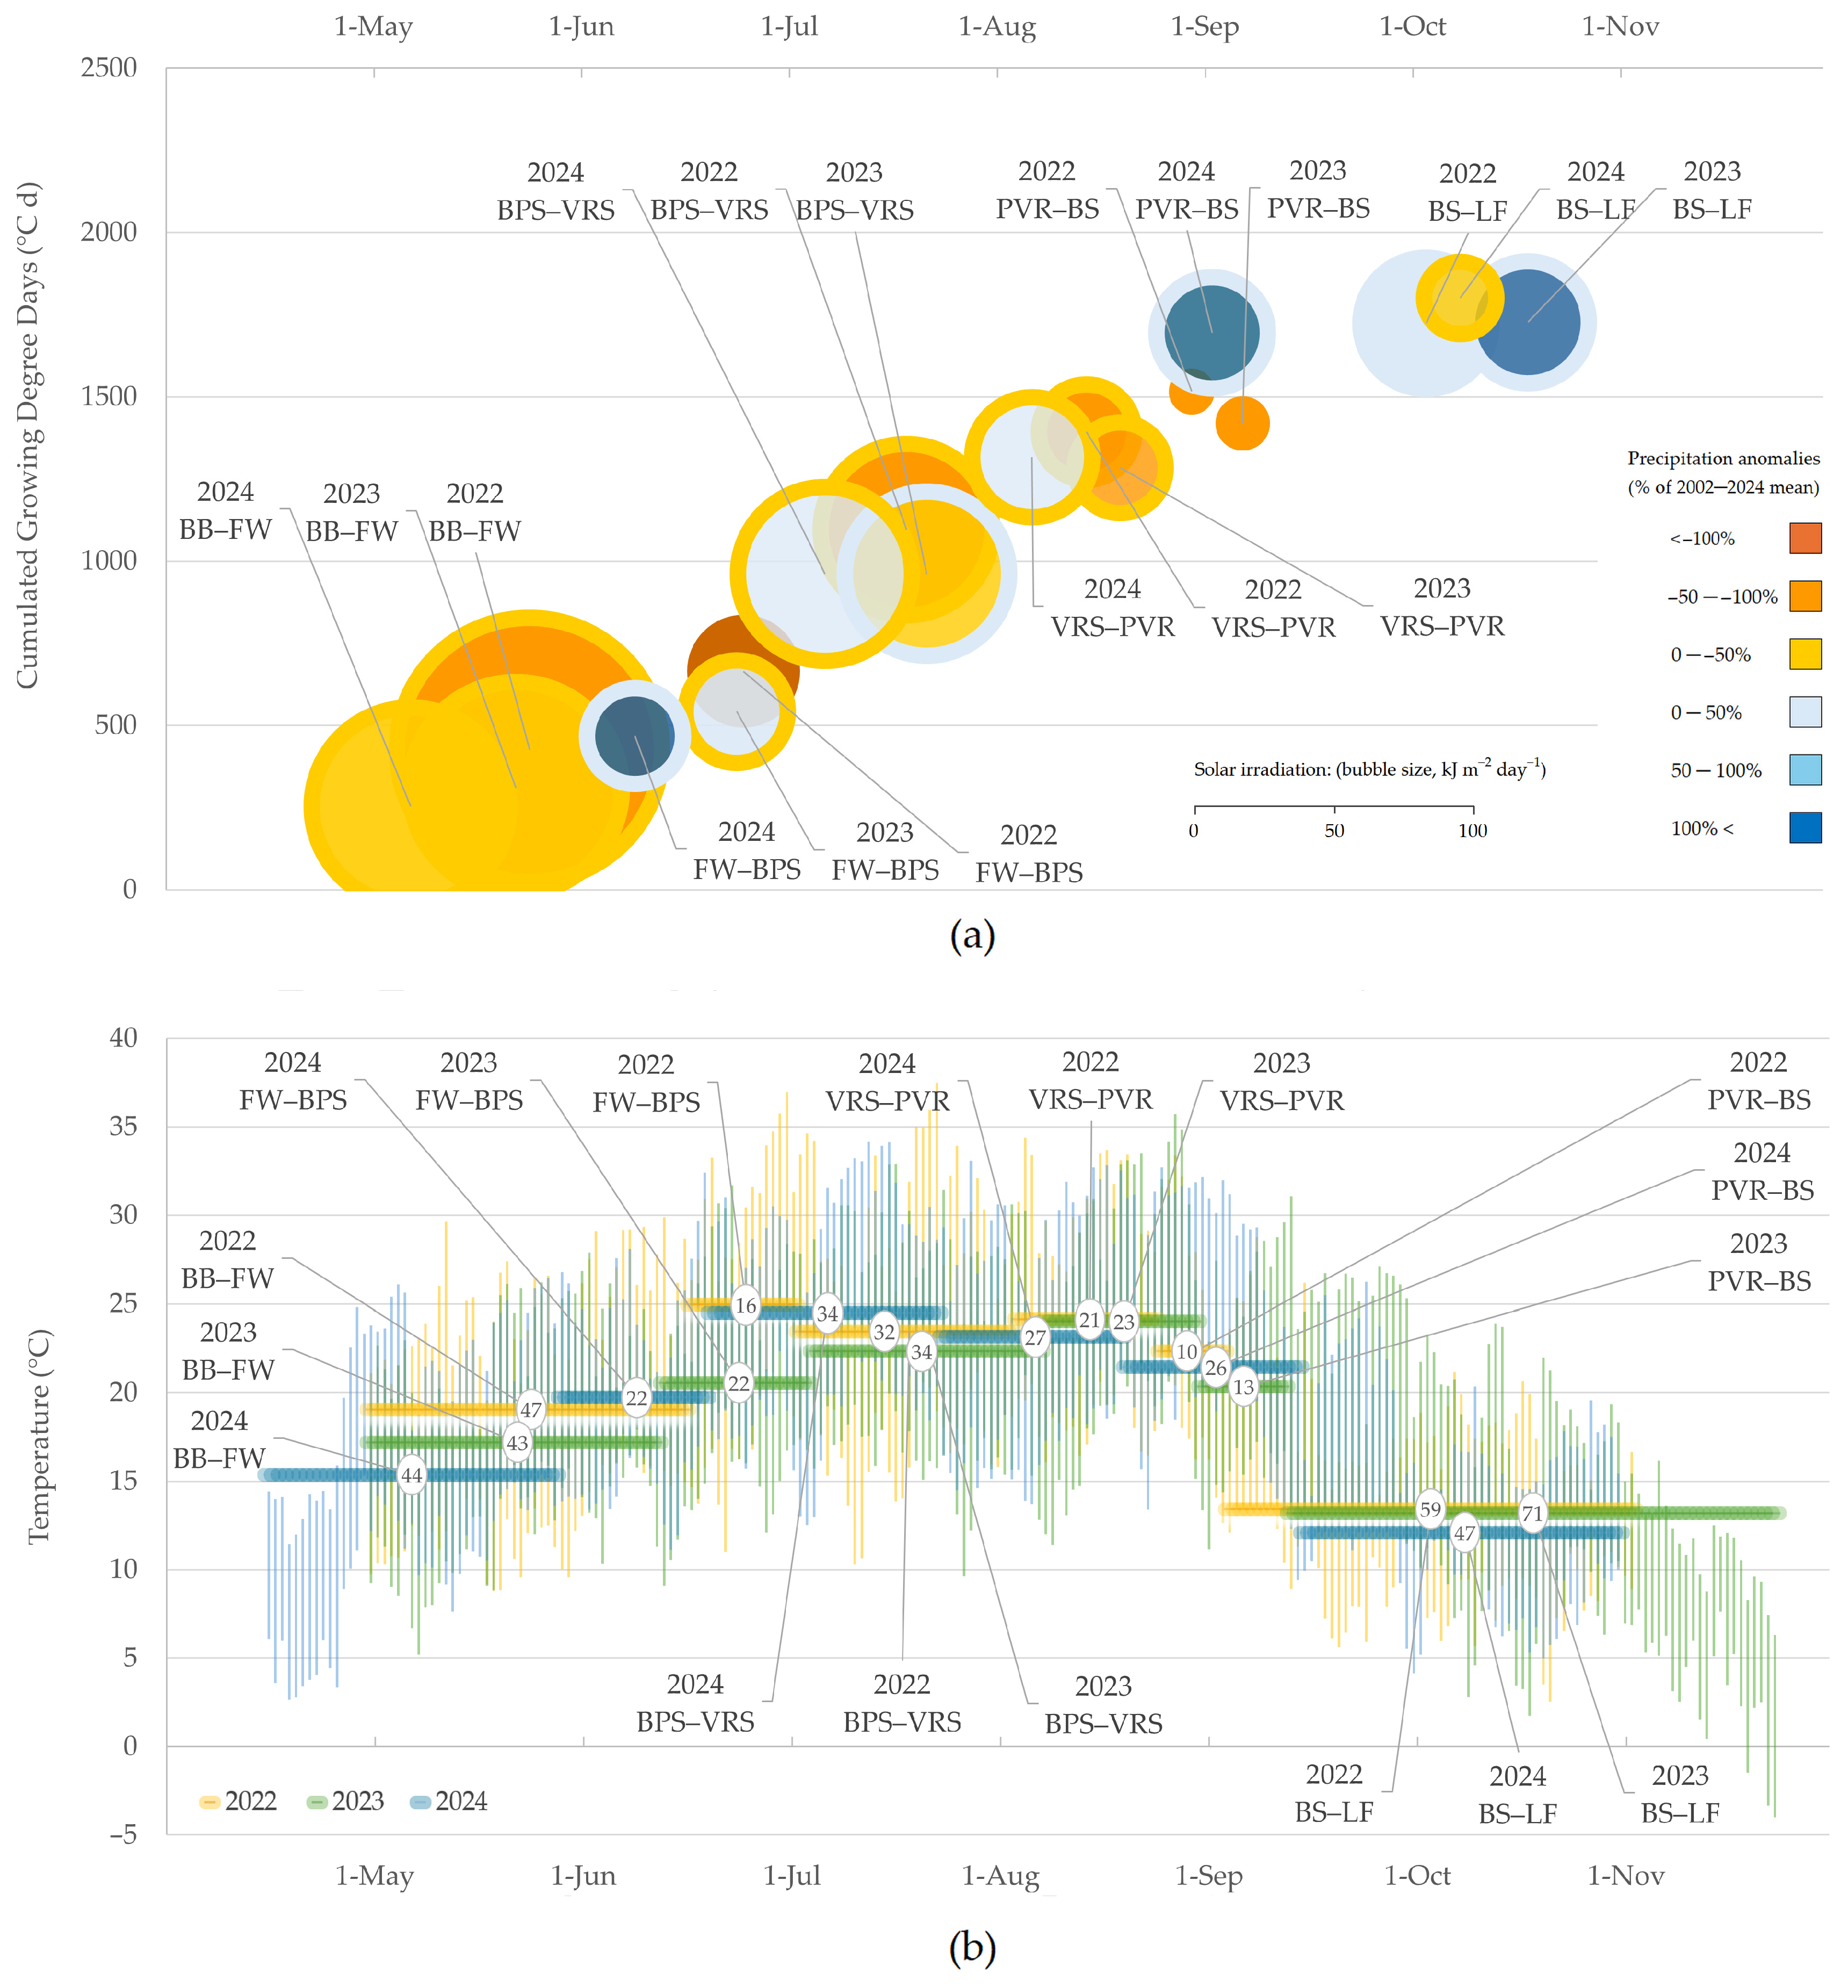
The three study years differed markedly in thermal load and water availability, providing a contrasting climatic framework for the interpretation of must composition.
  • The year 2022 was characterized by pronounced heat extremes and a prolonged early-season warm spell, during which daily maxima exceeded 37 °C. Night temperatures frequently remained below 15 °C during most of the vegetation period, resulting in large diurnal shifts. This year also stood out as the driest: both total rainfall and the number of rainy days were far below long-term averages, and most phenological intervals received minimal precipitation.
  • The year 2023 exhibited more moderate thermal conditions, heat accumulation (GDD, Winkler Index) remained close to the long-term norm. Rainfall gradually decreased after flowering resulting in a dry mid-season following a slightly wetter early season. Abundant post-sampling rainfall did not influence berry development and quality.
  • The year 2024 showed the greatest overall heat accumulation. Both GDD and the Huglin Index reached values notably exceeding long-term means, and solar irradiation sums were elevated during several phenological periods. Rainfall was abundant early in the season making 2024 the wettest pre-véraison year, yet water availability decreased during véraison before another increase toward ripening and sampling (Figure 2).
Taken together, the vintages represent a gradient from hot–dry (2022) through moderate–wet late season (2023) to hot–wet early season (2024), providing an ideal framework to isolate and evaluate the specific impacts of individual climate parameters on acidity, pH, mineral cations and phenolic composition.

3.2. Vintage Effects on Must Parameters

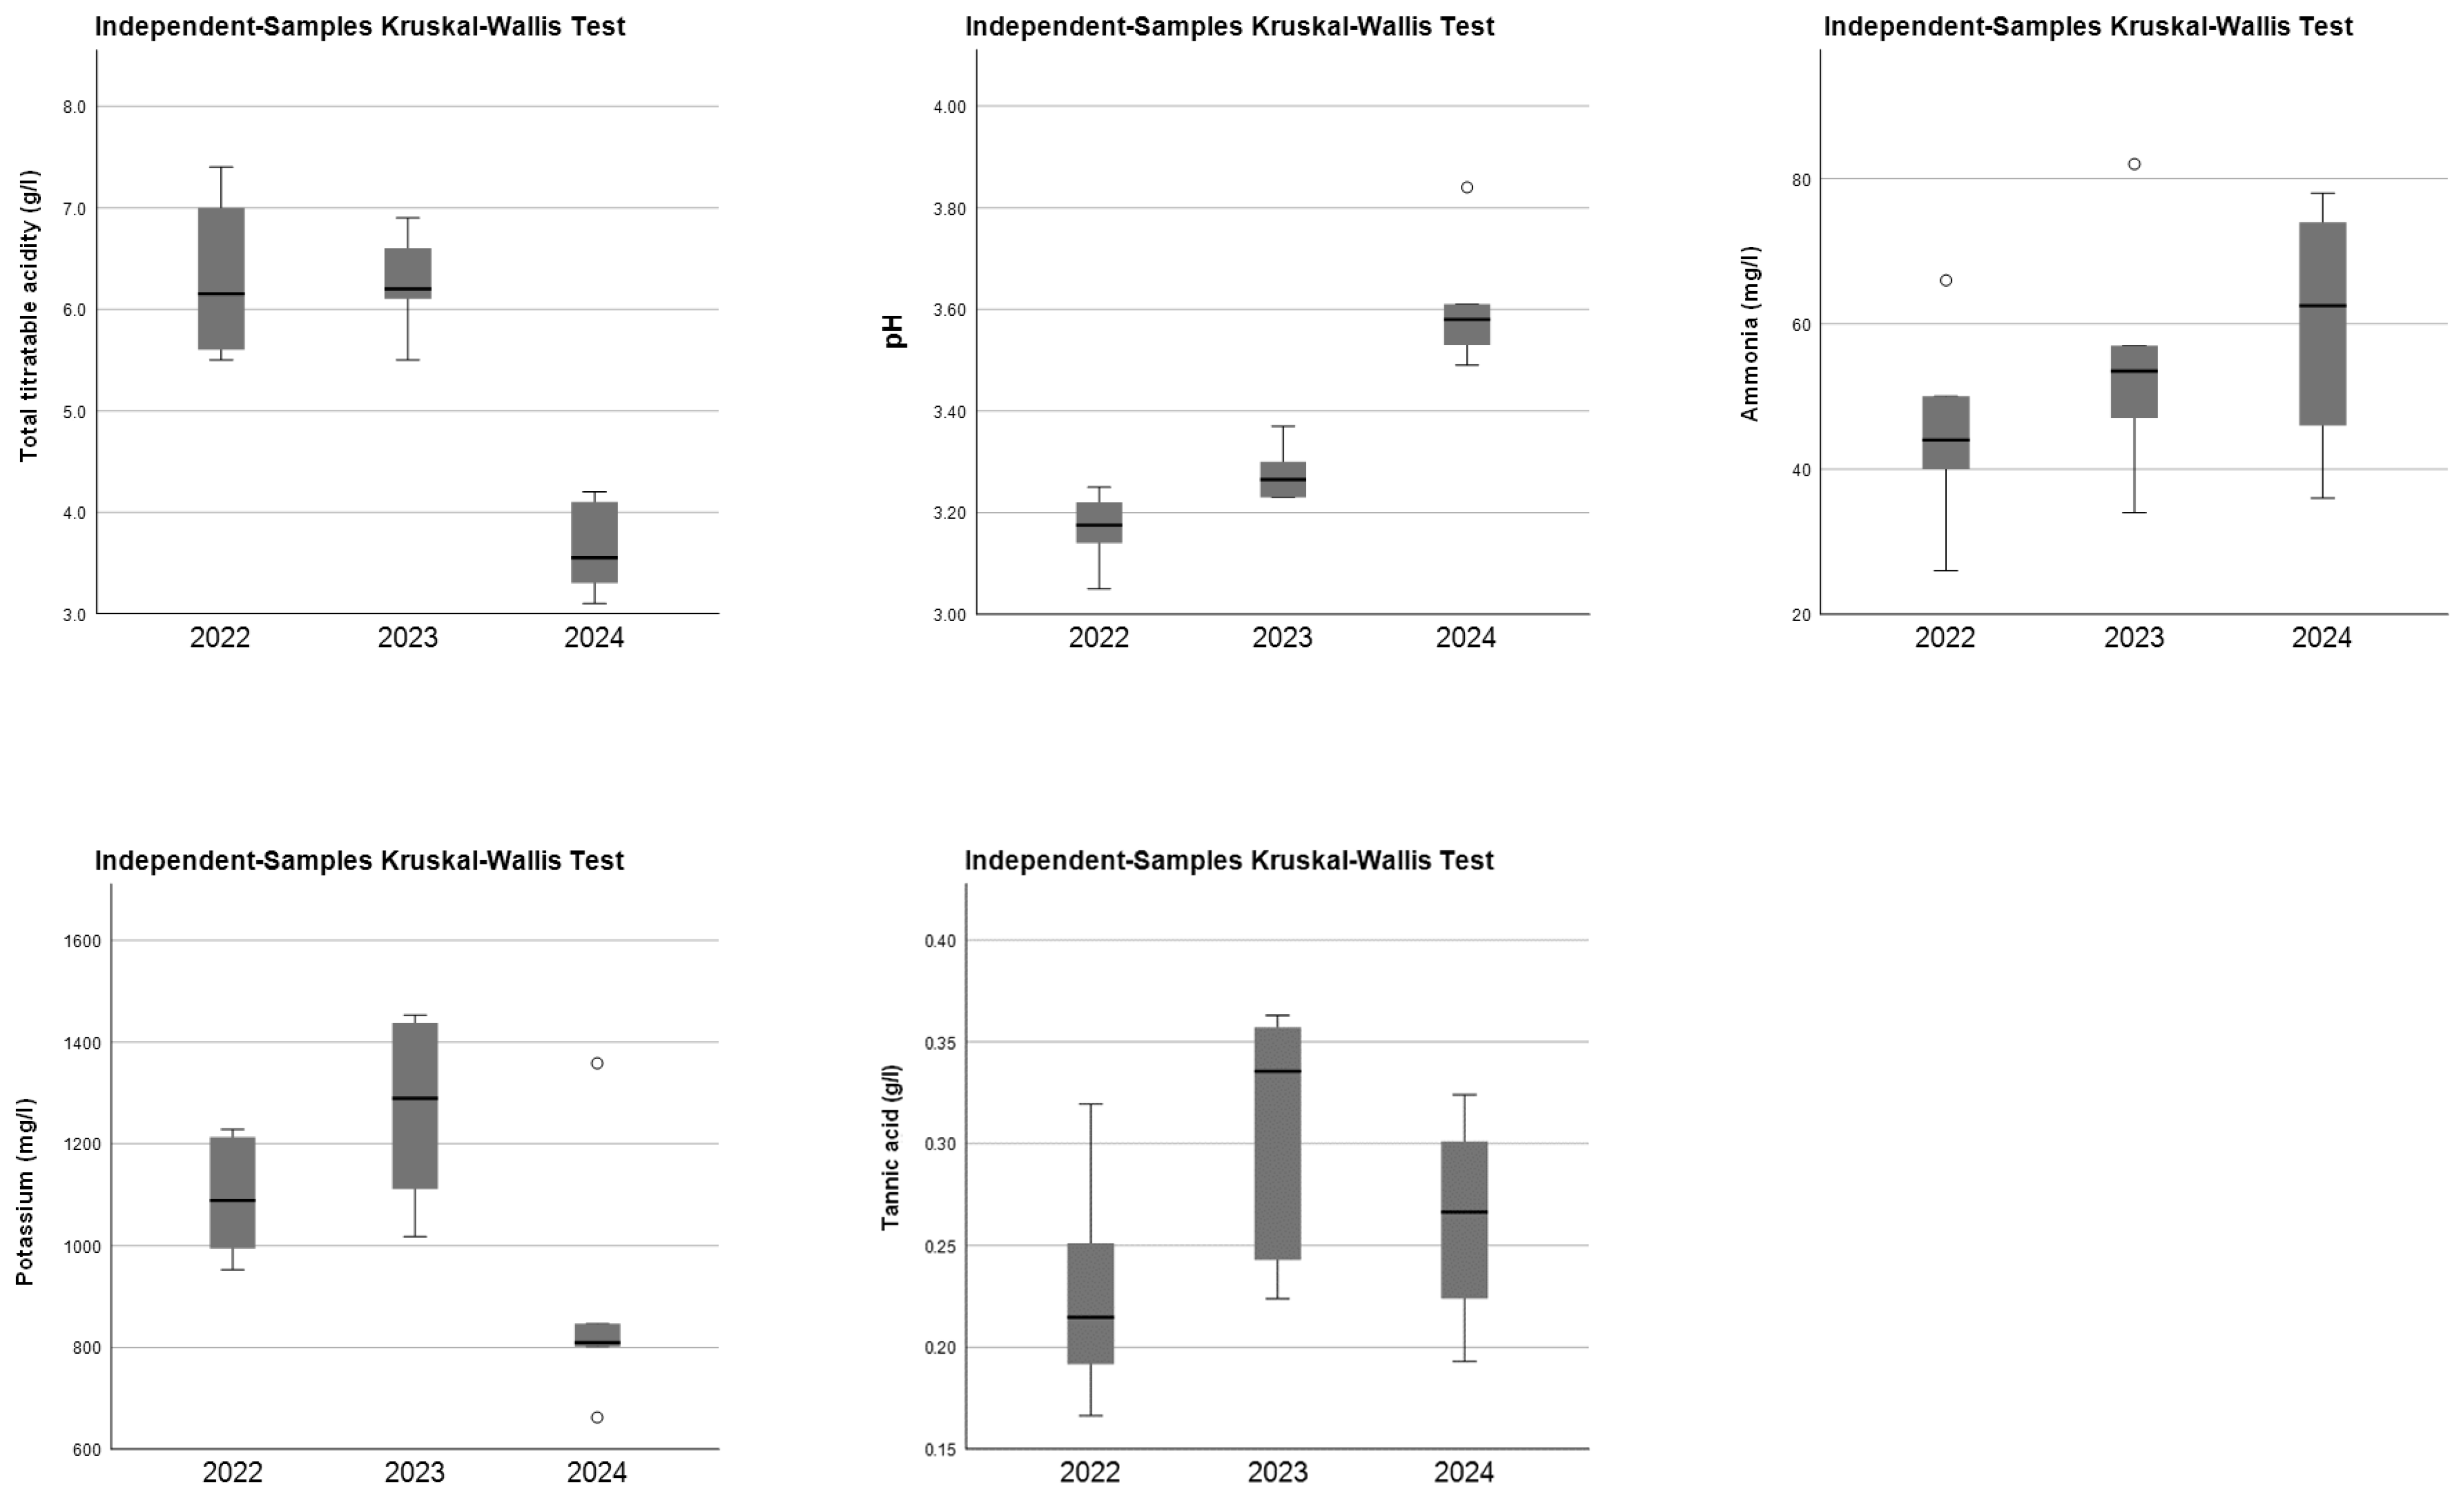
The Kruskal–Wallis test revealed significant interannual differences for several must components (Table 1).
Titratable acidity differed strongly among vintages (p < 0.01), with 2024 showing the lowest values—consistent with its elevated heat accumulation that could not be counteracted by the relatively good water supply.
Must pH also varied significantly (p < 0.01), displaying the expected inverse pattern relative to acidity: the warmest vintage (2024) had the highest pH.
Potassium concentration (K) showed significant vintage dependence (p < 0.05). Surprisingly, 2024 exhibited a notable decrease in K, despite conditions usually associated with enhanced potassium accumulation. This anomaly likely reflects site-specific differences in soil water status and ion mobility late in the season, as it is implied by the high variability among the six locations: under severe drying, restricted mass flow may override the physiological tendency for rising K concentrations.
Ammonia and tannic acid TAE showed weaker vintage discrimination; variations were present but did not follow a single, consistent climatic pattern across all sites.
Overall, acidity, pH and potassium showed the clearest year-to-year shifts, while ammonia and tannic acid displayed more muted vintage sensitivity.

3.3. Climatic Descriptors of Must Composition

A refined subset of climatic variables (those exhibiting both significant vintage effects and the closest correlations with must traits) was used to identify potential predictors (Table 2, Table 3, Table 4, Table 5 and Table 6). Below, only the principal patterns are summarized.

3.3.1. Titratable Acidity

Acidity was influenced by both thermal and water-supply factors.
Negative associations were found with:
  • Extreme rainfall days in July (and heavy rainfall days from June to August in slightly weaker correlations);
  • The frequency of tropical nights between pea-size and véraison;
  • The number of summer days from véraison to maturity.
This pattern is similar to the typical dilution-driven decrease seen in wetter years; however, the physiological background may differ. Conversely, increased heat load (average and maximum temperature, or cumulative heat units) during early stages tended to raise acidity. In Furmint, heat accumulation dynamics, from early season onwards, seemed to affect late-season organic acid content (Table 2).

3.3.2. pH

Climate-associated variables of pH were more numerous and generally stronger than those for acidity, despite the direct connection (inverse proportionality) between the two parameters.
pH decreased with:
  • Extreme heat days;
  • Cumulative heat units (GDD, BEDD);
  • High maximum temperatures during early development.
pH increased with:
  • Heavy rainfall episodes in June;
  • Elevated late-season solar irradiation.
Thus, pH integrates both water and thermal stress signals but is particularly sensitive to early-season heat load and, in general, high extremes in temperature (Table 3).

3.3.3. Ammonia

Correlations with climatic variables were mostly weak to moderate. The most prominent climate-associated variables were:
  • The highest nightly minimum temperatures in May;
  • The number of heavy rainfall days from May to pea-size.
Most associations were positive, suggesting that warm, moist early-season conditions promote higher ammonia content, though heat extremes had only minor explanatory power (Table 4).

3.3.4. Potassium

Potassium (K+) concentration showed moderate associations with night-time and late-season climatic conditions.
K increased with:
  • The number of tropical nights (véraison–maturity);
  • Higher daily mean temperatures;
  • Rainfall days in July.
Negative correlations were found with:
  • Hot days;
  • Summer days;
  • Cumulative heat units;
  • The minimum of daily mean temperatures.
These patterns indicate that potassium accumulation is enhanced under temperate to warm, humid mid-season conditions but may be suppressed when high heat coincides with reduced water availability (Table 5) which heavily modulates the rate of phloem potassium loading across specific post-véraison phenological stages. This dual response highlights a clear asymmetry between moderate macroclimatic configurations and extreme thermal events. While regular July rainfall combined with warm ambient temperatures provides optimal conditions for metabolic activity and potential soil-to-root mass flow, excessive heat accumulation (reflected in the negative trends with summer days and cumulative heat units) acts as a limiting factor. This suggests that the physiological mechanisms driving final must potassium concentrations are highly sensitive to the balance between atmospheric evaporative demand and moisture availability during the core ripening window.

3.3.5. Tannic Acid (TAE)

Tannic acid exhibited the second-highest number (20) of valid climatic variables, surpassed only by pH.
Strikingly, all correlations were negative, irrespective of the type of climatic variable:
  • Maximum temperature (strongest group of correlated variables);
  • Mean temperature;
  • Heat units (GDD, BEDD);
  • Solar irradiation;
  • Early season diurnal temperature range.
This suggests that spatial variations in thermal and radiation stress are associated with reduced TAE levels, either through altered biosynthesis, degradation, or shifts in berry structure affecting extractability (Table 6).

3.4. Summary of Climatic Sensitivity

Across traits, the strongest climate–must relationships were observed for:
  • pH and acidity (most robust and diverse set of candidate correlates);
  • Tannic acid (second highest number of associated variables);
  • Potassium (few but relatively strong correlates).
Ammonia was the least climate-sensitive parameter in this dataset.
Generally, early phenological periods (bud burst to pea-size) emerged as the most decisive windows for climate–must interactions, although the sensitivity observed during these stages likely reflects predominantly indirect effects mediated through phenological timing and canopy development rather than direct biochemical control. Extreme heat events, night-time temperatures, and rainfall anomalies were the dominant climatic factors shaping compositional outcomes. Specifically, acidity-related traits exhibited the highest dependence on the bud burst to pea-size interval (6–9 candidate correlates), followed by a secondary surge in correlation frequency (4–5) during the véraison to berry sampling window. Ammonia levels were primarily associated with the flowering to véraison stage (5 variables) and the period immediately preceding harvest (2 varaibles), while potassium sensitivity was clearly restricted to the pea-size to post-véraison interval (4 variables). For tannic acid, although correlates were distributed evenly across phenophases from flowering to post-véraison, calendar-based aggregation shifted this focal point to May and June. While monthly summaries generally aligned with phenological trends for most parameters, they proved less effective at capturing the secondary sensitivity peak in late phenological stages, where the number of valid climate-associated variables for acidity, ammonia, and potassium notably increased.

4. Discussion

4.1. Total Acidity and pH

High to extremely high temperatures, increased solar radiation, and limited water availability are widely recognized as major drivers of acidity loss in grape must, whereas cooler and more humid conditions generally preserve acidity [13,14,15,16,17]. Viticultural practices may substantially modify these climatic influences [18]. In Furmint, titratable acidity exhibited a clear decline with the frequency of mid-season warm nights (≥20 °C) and moderately warm days (≥25 °C). By contrast, early-season biologically effective degree days (BEDD) and average daily peak temperatures showed weaker positive associations with acidity, which is consistent with the structure of BEDD, as this index excludes the contribution of extreme heat.
Previous findings linking acidity to mean temperature anomalies [19,20], phenological timing [21], and diurnal temperature dynamics [22] were only partially corroborated. The physiological basis for these observations likely aligns with established grapevine responses: elevated temperatures are widely reported to accelerate ripening and drive malic acid depletion, while tartaric acid remains comparatively temperature-stable [23,24]. Although individual organic acids were not quantified in the present study—preventing the direct decoupling of malic acid degradation, tartaric acid dynamics, or specific buffering pathways—historical literature suggests that, individual organic acids often display distinct climatic sensitivity [20]. As expected from the tight mechanistic coupling between acidity and pH, the temperature response of pH closely mirror-images that of organic acids confirming the internal consistency of our microclimatic models.
Notably, several pH-related responses in Furmint diverged from those typically observed in other cultivars. A higher frequency of extreme heat events (≥35 °C) and elevated late-season maximum temperatures corresponded to lower pH values. Similarly, BEDD, GDD, and early-season peak temperatures exhibited negative associations with pH. In contrast, frequent June rainfall events and increased post-véraison irradiation contributed to higher must pH, in line with the moderate negative relationship between extreme rainfall and acidity. While these patterns remain preliminary observations specific to this dataset, they suggest a hypothesis that Furmint may possess distinct acid-retention tendencies under specific thermal conditions. Genotype-, ripening-stage-, and region-specific responses to climate are well documented [25,26,27]. If verified via comparative cultivar trials across longer time series, these tentative trends could point toward genetic attributes of Furmint that are highly relevant in the context of ongoing climatic warming [28]. Furthermore, effectively decoupling these atypical pH and acidity responses will require the separate quantification of individual organic acids (such as tartaric and malic acids) in future trials, given their differing thermal stabilities.

4.2. Ammonia Content

Ammonia levels in grape must exhibit marked climatic sensitivity, with temperature and precipitation acting as principal determinants. Cool-climate regions—where the warmest-month mean remains below 20.7 °C—commonly show elevated ammonium concentrations due to prolonged maturation and reduced metabolic degradation [29,30]. Warmer climates accelerate ammonia depletion through intensified metabolic deamination and enhanced volatilization [31]. Extreme heat (>35 °C) combined with water deficit further restricts nitrogen uptake, reducing ammonium accumulation by limiting root absorption and internal partitioning [32]. Enhanced nitrogen uptake under cooler conditions can increase berry nitrogenous compounds, leading to higher must ammonia levels [33,34]. Precipitation modifies these processes, with wetter conditions elevating ammonium content through delayed ripening and reduced degradation [30]. Additionally, ammonia formation from amino acid degradation may contribute to must nitrogen levels [35]. Given ammonia’s strong influence on fermentation dynamics—and its interaction with must pH—these climatic sensitivities have meaningful oenological implications, especially in warm regions where ammonia-induced alkalinization may intensify. However, since free amino nitrogen (FAN) was not determined in this study, these trends reflect only the inorganic fraction of yeast-assimilable nitrogen.
In the present study, interannual variation in ammonia content was modest, with slightly increasing levels across the vintages. Ammonia was positively associated with higher daily minima and mean temperatures during early phenological stages, whereas heat days showed weak negative relationships. Heavy rainfall events early in the season increased ammonium ion concentrations, and overall water availability supported elevated levels throughout the growing period.
The limited climatic sensitivity observed here may indicate that Furmint regulates nitrogen metabolism more conservatively under thermal stress than other cultivars. These findings contrast with the pronounced vintage effects reported in other cool- and warm-climate viticultural studies and suggest that soil N status or genotype-specific nitrogen partitioning may play a more dominant role than climate in determining Furmint ammonia levels.

4.3. Potassium Content

Potassium typically exhibits a negative association with acidity in grape must, and its accumulation is primarily regulated by temperature in the ripening stage. During berry development, higher temperatures enhance potassium translocation from vegetative tissues while diminishing photosynthetic activity [36]. Increasing potassium levels contribute to malic acid degradation and tartaric acid precipitation through potassium bitartrate formation. Under cooler thermal regimes, however, shifts in pH may be driven predominantly by potassium transport rather than organic acid loss [37]. Previous research suggests that soil potassium content and climatic variables such as rainfall, humidity, and solar radiation exert weaker effects on berry potassium concentrations than temperature, genotype, and viticultural practices [38,39].
Furmint slightly deviated from the established patterns. The candidate climatic predictors identified for potassium concentration largely reflected the factors influencing acidity in an inverse manner, consistent with the widely documented negative correlation between these parameters [40,41,42,43,44]. Specifically, potassium accumulation was promoted by daily average temperatures, July rainfall, and late-season tropical nights, while being restricted by early-season hot days, mid-season GDD, and high daily minimum temperatures. However, a notable discrepancy was observed in the 2024 vintage. Despite 2024 being the warmest and wettest year with high solar radiation—conditions that included several favorable factors for potassium accumulation (e.g., late tropical nights, July rainfall)—both potassium and acidity levels remained low. This simultaneous decline presents an intriguing observation, potentially suggesting a decoupling of the standard potassium-acidity relationship under the extreme conditions of 2024. Because vine water status, soil moisture, and leaf or soil mineral composition were not monitored continuously in this study, the exact underlying physiological mechanisms cannot be verified. Therefore, this pattern remains a preliminary observation contrasting with some earlier findings regarding environmental impacts on potassium [38,45,46,47,48] and necessitating further investigation into the cultivar-specific physiological responses of Furmint.

4.4. Tannic Acid Content

Tannin concentrations in white wines are substantially lower than in red varieties owing to varietal characteristics and winemaking processes, as tannins are predominantly located in the berry skin [49,50]. Tannin accumulation generally increases throughout ripening; consequently, climatic conditions that accelerate ripening—such as elevated temperatures, higher GDD accumulation, and increased solar radiation—are usually positively correlated with tannin content [51]. Mild positive associations with nocturnal cooling, effective heat accumulation, and sunshine duration have also been reported, whereas precipitation often shows a weak negative relationship with tannin formation [20]. Excessively high temperatures, however, may disrupt phenolic biosynthesis and reduce phenolic concentrations [52,53].
Across the examined vintages, tannic acid concentration in Furmint must exhibited limited interannual variability at the vintage level (Table 2). Most thermal variables—including peak temperatures, diurnal temperature range and cumulative heat—and solar irradiation were negatively associated with tannin levels, albeit typically with weak to moderate strength. No meaningful relationships were observed with water availability indicators. These findings diverge from patterns reported in other cultivars and terroirs [20,51,54,55]. This disparity underscores that while macro-climatic annual shifts were minor, spatial topoclimatic gradients across different elevations within the vineyard may heavily influence tannin accumulation. Given the limited number of vintages, statistical anomalies cannot be completely ruled out at this stage. Nevertheless, as this study is part of an ongoing, long-term monitoring project, capturing a broader multi-year dataset is expected to allow for the formal decoupling of these seasonal and topo-climatic effects, which remains a key priority for future research. The consistently low tannin concentrations typical of Furmint must may partly account for these limited associations, and the relative infrequency of extreme heat events during the study period likely further reduced the expression of climatic sensitivity. Given the incomplete understanding of thermal regulation of tannin biosynthesis in white cultivars, further research is clearly warranted [56,57].

4.5. Key Implications

This study highlights potential cultivar-specific climatic sensitivities in Furmint must composition, revealing distinct thermal and hydrological associations with acidity, pH, potassium, ammonia and tannin responses. The findings provide a theoretical framework for optimizing vineyard management strategies under warming and increasingly variable climatic conditions and establish a framework for further in-depth analyses.
  • Furmint must composition exhibits distinct trends that appear to diverge from patterns commonly reported for other white varieties.
  • Acidity and pH show atypical responses to heat, suggesting an intriguing acid-retention capacity and possible adaptive potential under warming conditions which warrants further validation in comparative trials.
  • Potassium and acidity may change together, suggesting a partial decoupling of classical K–acid mechanisms under extreme conditions.
  • Ammonia responds weakly to climatic variation, highlighting the likely dominant role of genotype and soil N status.
  • Tannic acid decreases under all thermal intensities, indicating limited phenolic resilience in this dataset.
  • These results emphasize the importance of developing variety-specific climate sensitivity matrices for future climate-adaptive viticulture in Tokaj and similar continental regions.

5. Conclusions

This study provided a comprehensive analysis of annual variability in Furmint grape must composition and its dependence on climatic factors underlying the vintage effect in the Tokaj wine region. While some must parameters exhibited a clear vintage effect, linked to interannual differences in temperature and rainfall, not all parameters responded to changes in climate. Moreover, the most influential climatic factors identified in this study occasionally diverged from previous findings, particularly for pH, potassium content, and tannin content.
These contradictory or unexpected results warrant further confirmation through extended studies, both in terms of duration and the range of parameters assessed. Future work should prioritize the detailed analysis of grape organic acids, evaluating the relationships between specific acids—such as malic, tartaric, and citric acid—and climatic variables, given their distinct stabilities with respect to temperature and water availability [58,59,60].
While this study utilized a comprehensive set of thermal, radiation, and water-related indices, incorporating atmospheric humidity and evapotranspiration could further refine the understanding of crop water budgets under climate stress. Accordingly, ongoing research within this project is already expanding to integrate soil properties and mineral dynamics—specifically potassium—to fully elucidate the multi-layered interactions shaping Furmint must composition within the dynamic vineyard environment.

Author Contributions

Conceptualization, A.C.D. and I.S.; methodology, A.C.D., C.R. and K.M.; software, T.D.-N.; validation, C.R. and K.M.; formal analysis, C.R. and K.M.; investigation, C.R., K.M., K.B., I.K. and A.C.D.; resources, A.C.D.; data curation, C.R., K.M., K.B. and I.K.; writing—original draft preparation, C.R.; writing—review and editing, C.R., T.D.-N., and A.C.D.; visualization, A.C.D.; supervision, L.C.; project administration, A.C.D., I.S. and L.C.; funding acquisition, L.C. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by National Research, Development, and Innovation Fund of Hungary project no. 2018-1.2.1-NKP-2018-00002, GINOP-2.2.1-15-2016-00021 and GINOP-2.2.1-15-2017-00076.

Data Availability Statement

The datasets presented in this article are not readily available because the data are part of an ongoing study.

Conflicts of Interest

The authors declare no conflicts of interest. The funders had no role in the design of the study; in the collection, analyses, or interpretation of data; in the writing of the manuscript; or in the decision to publish the results.

Appendix A

Table A1. Overview of the time-specific climatic parameters and bioclimatic indices categorized by time windows. (Adapted from [1]).
Sap Flow RelatedPhenology Related PeriodsCalendar MonthsCustom Periods for Specific Indices
Climatic Parameters/IndicesSapFlow Bud Burst—Berry SamplingSapFlow Bud Burst—Leaf FallBlooming Period (15 May–15 June)Ripening Period (1 June–30 September)Harvest Time (15 August–15 October)AprilMayJuneJulyAugustSeptemberOctoberNovemberMarch–MayApril–SeptemberApril–OctoberJune–SeptemberJune–AugustSeptember–November
Huglin’s Heliothermic Index
Winkler index
Cool Night Index
No. of Tropical Nights
No. of Summer Days
No. of Hot Days
No. of Extremely Hot Days
GS Average Temperature
GS Minimum Temperature
GS Maximum Temperature
GS Thermal Amplitude
Harvesttime Max. Temperature
Harvesttime Min. Temperature
Harvesttime Thermal Amplitude
Mean July monthly Avg. Temp.
July Diurnal Range
Ripening Avg Temperature
Number of Spring Frost Days
Sum of Spring Freezing Temps
Number of Fall Frost Days
Sum of Fall Freezing Temps
Growing Season Rainfall
Growing Season Rainy Days
Summer Rainfall
Blooming Period Rainfall
Ripening Period Rainfall
Ribéreau-Gayon-Peynaud Index
Dunkel’s Radiothermal Index
Time window specifications are provided for each individual parameter. Shading marks the parameter–period pairings used in the subsequent analysis.
Table A2. Overview of climatic variables not restricted to specific phenological timings. (Adapted from [1]).
Actual Phenological StagesSap Flow RelatedPhenology Related PeriodsCalendar Months
Climatic Parameters/IndicesBud Burst—FloweringFlowering—Berries Peas SizeBerries Pea-Size—VéraisonVéraison—Post VéraisonPost-Véraison—Berry SamplingBerry Sampling—Leaf FallBud Burst—Leaf FallBud Burst—Berry SamplingBud Burst—End of Sap FlowSapFlow Bud Burst—Berry SamplingSapFlow Bud Burst—Leaf FallBlooming Period (15 May–15 June)Ripening Period (1 June–30 September)Harvest Time (15 August–15 October)AprilMayJuneJulyAugustSeptemberOctoberNovember
Growing Degree Days
Biologically Effective Degree Days
Minimum Temperature (Minimum)
Minimum Temperature (Average)
Minimum Temperature (Maximum)
Mean Temperature (Minimum)
Mean Temperature (Average)
Mean Temperature (Maximum)
Maximum Temperature (Minimum)
Maximum Temperature (Average)
Maximum Temperature (Maximum)
Minimum Temperature > 20 °C
Maximum Temperature ≥ 25 °C
Maximum Temperature ≥ 30 °C
Maximum Temperature ≥ 35 °C
Diurnal Range of Temperature
Minimum Temp. < 0 °C (Frost Days)
Freezing Degree Days
Heavy Rainfall Days (R ≥ 10 mm)
Extreme Rainfall Days (R ≥ 20 mm)
Sum of Global Irradiation
Average Daily Irradiation
High Global Irr. Days (SR > 2.5 kJ)
Highest Daily Irradiation
Time window specifications are provided for each individual parameter. Shading marks the parameter–period pairings used in the subsequent analysis.

Appendix B

Table A3. Definition and methodology of the bioclimatic parameters (Adapted from [1]).
ParameterAbbr.FormulaReferences
Growing Degree Days 1–11,18–20 [°C]GDD m a x T A V G 10 ; 0 [60]
Absolute Minimum Temp. 1–11 [°C]MIN TMIN m i n T M I N -
Average Minimum Temp. 1–11 [°C]AVG TMIN a v g T M I N -
Maximal Minimum Temp. 1–11 [°C]MAX TMIN m a x T M I N -
Minimum of Mean Temp. 1–11 [°C]MIN TAVG m i n T A V G -
Average of Mean Temp. 1–11 [°C]AVG TAVG a v g T A V G -
Maximum Mean Temp. 1–11 [°C]MAX TAVG m a x T A V G -
Minimal Maximum Temp. 1–11 [°C]MIN TMAX m i n T M A X -
Average Maximum Temp. 1–11 [°C]AVG TMAX a v g T M A X -
Absolute Maximum Temp. 1–11 [°C]MAX TMAX m a x T M A X -
Number of Tropical Nights 1–11,14 [day]NTN c o u n t T M I N d a y 20   ° C -
No. of Summer Days 1–11,14 [day]NSD c o u n t T M A X d a y 25   ° C -
No. of Hot Days 1–11,14 [day]NHD c o u n t T M A X d a y 30   ° C -
No. of Extremely Hot Days 1–11,14 [day]NEHD c o u n t T M A X d a y 35   ° C -
Diurnal Range of Temp. 1–11 [°C]DRT a v g T M A X d a y T M I N d a y -
Number of Frost Days 1–11 [day]NFD c o u n t T M I N d a y < 0   ° C -
Freezing Degree Days 1–11 [°C]FDD m i n T M I N ; 0 [61]
Rainfall Days 1–11 [day]RD c o u n t R a i n f a l l d a y > 0   mm -
Heavy Rainfall Days 1–11 [day]HRD c o u n t R a i n f a l l d a y 10   mm -
Extreme Rainfall Days 1–11 [day]ERD c o u n t R a i n f a l l d a y 20   mm -
Sum of Global Irradiation 1–11 [kJ m−2]IR G l o b a l   I r r a d i a t i o n -
Average Daily Irradiation 1–11 [kJ m−2]IRDAVG a v g G l o b a l   I r r a d i a t i o n d a y -
High Global Irrad. Days 1–11 [day]HIR c o u n t G l o b a l   I r r a d i a t i o n d a y 2.5   kJ · m 2 -
Max. Daily Irradiation 1–11 [kJ m−2]IRMAX m a x G l o b a l   I r r a d i a t i o n p e r i o d -
Biologically Effective. Degree Days 1–11,14,18–20 [°C]BEDD 1   A p r 31   O c t m a x m i n T A V G ; 19 10 ; 0 [62,63]
Huglin’s Heliothermic Index 13 [°C]HI 1   A p r 30   S e p m a x 0 ; T M A X 10 ; 0 + m a x 0 ; T A V G 10   2 · K [64]
Winkler Index 14 [°C]WI 1   A p r 31   O c t m a x T A V G 10 [65,66]
Cool Night Index 9 [°C]CNI a v g 1 30   S e p T M I N [67]
Growing Season Avg. Temp. 2,3,14 [°C]GSAT a v g 1   A p r 31   O c t T A V G [68]
G.S. Average Min. Temp. 2,3,14 [°C]GSATN a v g 1   A p r 31   O c t T M I N [68]
G.S. Avg. Maximum Temp. 2,3,14 [°C]GSATX a v g 1   A p r 31   O c t T M A X [68]
G.S. Diurnal Range 2,3,14 [°C]GSDR a v g 1   A p r 31   O c t T M A X T M I N -
Ripening Period Max. Temp. 15,20 [°C]RMX a v g 1   J u n 30   S e p T M A X [69]
Ripening P. Minimum Temp. 15,20 [°C]RMN a v g 1   J u n 30   S e p T M I N -
Ripening P. Diurnal Range 15,20 [°C]RDR a v g 1   J u n 30   S e p T M A X T M I N [70]
Mean July Temperature 7 [°C]MJT a v g 1 31   J u l T A V G [70]
July Diurnal Range 7 [°C]JDR a v g 1 31   J u l T M A X T M I N [71]
Ripening Average Temp. 20 [°C]RAT a v g 15   J u l 15   O c t T A V G [68]
No. of Spring Frost Days 12 [day]NSFD c o u n t 1   M a r 31   M a y T M I N d a y < 0   ° C -
Sum of Spring Freezing T. 12 [°C]SSFT 1   M a r 31   M a y m i n T M I N ; 0 -
Number of Fall Frost Days 17 [day]NFFD c o u n t 1   S e p 30   N o v T M I N d a y < 0   ° C -
Sum of Fall Freezing Temps. 17 [°C]SFFT 1   S e p 30   N o v m i n T M I N ; 0 -
Growing Season Rainfall 2,3,14 [mm]GSR 1   A p r 31   O c t R a i n f a l l [72,73]
Growing Season Rainy Days 2,3,14 [day]GSRD c o u n t 1   A p r 31   O c t R a i n f a l l d a y > 0   mm -
Summer Rainfall 16 [mm]SR 1   J u n 31   A u g R a i n f a l l [74]
Bloom Period Rainfall 18 [mm]BR 15   M a y 15   J u n R a i n f a l l -
Ripening Period Rainfall 20 [mm]RR 15   A u g 15   O c t R a i n f a l l [75]
Ribéreau-Gayon-Peynaud Ind. 2,3,14 [–]RGPI 1   A p r 31   O c t m a x T A V G d a y 10 ; 0 R a i n f a l l d a y [76]
Dunkel’s Radiothermal Index 2,3,14 [–]DRI A · G n · 10 2 [77]
Abbreviations: avg, min, and max denote average, minimum, and maximum values, respectively. The latitude-adjustment constant for the Huglin Index (HI) is K = 1.05. Within the Dunkel’s Radiothermal Index (DRI) formula, A represents Growing Degree Days (°C), G indicates global irradiation (Jcm−2), and n signifies the growing season length (days). All indices are derived from daily aggregated datasets, with units specified in square brackets. Numerical codes (1–20) represent specific temporal windows: 1 phenological stages; 2 bud burst to sampling; 3 bud burst to leaf fall; 4−11 individual months from April to November; 12 March–May; 13 April–September; 14 April–October; 15 June–September; 16 June–August; 17 September–November; 18 bloom period (15 May–15 June); 19 ripening (1 June–30 September); 20 harvest (15 August–15 October).

Appendix C

Figure A1. Distribution of must quality parameters (2022–2024) shown as boxplots (n = 30 per annum). The median is denoted by the horizontal line within the box (interquartile range, IQR). Whiskers represent the spread of data up to 1.5 × IQR, while individual points (circles) beyond the whiskers indicate statistical outliers. (Adapted from [1]).
Agronomy 16 01253 g0a1

References

  1. Rácz, C.; Molnár, K.; Dövényi-Nagy, T.; Bakó, K.; Kathy, I.; Szepsy, I.; Csige, L.; Dobos, A.C. Cultivar-Specific Expression of the Vintage Effect in Furmint Grapes from the Tokaj Wine Region Part I: Berry Growth, Sugar Accumulation and Dry Matter Formation. Agronomy 2026, 16, 594. [Google Scholar] [CrossRef] [Scilit]
  2. Poni, S.; Gatti, M.; Palliotti, A.; Dai, Z.; Duchêne, E.; Truong, T.T.; Ferrara, G.; Matarrese, A.M.S.; Gallotta, A.; Bellincontro, A.; et al. Grapevine quality: A multiple choice issue. Sci. Hortic. 2018, 234, 445–462. [Google Scholar] [CrossRef] [Scilit]
  3. van Leeuwen, C.; Darriet, P. The impact of climate change on viticulture and wine quality. J. Wine Econ. 2016, 11, 150–167. [Google Scholar] [CrossRef] [Scilit]
  4. Naulleau, A.; Gary, C.; Prévot, L.; Hossard, L. Evaluating Strategies for Adaptation to Climate Change in Grapevine Production–A Systematic Review. Front. Plant Sci. 2021, 11, 607859. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Costa, E.; Cosme, F.; Jordão, A.M.; Mendes-Faia, A. Anthocyanin Profile and Antioxidant Activity from 24 Grape Varieties Cultivated in Two Portuguese Wine Regions. OENO One 2014, 48, 51–62. [Google Scholar] [CrossRef] [Scilit]
  6. Villette, J.; Cuéllar, T.; Verdeil, J.L.; Delrot, S.; Gaillard, I. Grapevine Potassium Nutrition and Fruit Quality in the Context of Climate Change. Front. Plant Sci. 2020, 11, 123. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Bisson, L. Yeast and Biochemistry of Ethanol Formation. In Principles and Practices of Winemaking; Boulton, R.B., Singleton, V.L., Bisson, L.F., Kunkee, R.E., Eds.; Chapman & Hall: New York, NY, USA, 1996; pp. 140–172. [Google Scholar]
  8. Bouloumpasi, E.; Skendi, A.; Soufleros, E.H. Survey on Yeast Assimilable Nitrogen Status of Musts from Native and International Grape Varieties: Effect of Variety and Climate. Fermentation 2023, 9, 773. [Google Scholar] [CrossRef] [Scilit]
  9. Berli, F.; D’Angelo, J.; Cavagnaro, B.; Bottini, R.; Wuilloud, R.; Silva, M.F. Phenolic Composition in Grape (Vitis vinifera L. cv. Malbec) Ripened with Different Solar UV-B Radiation Levels by Capillary Zone Electrophoresis. J. Agric. Food Chem. 2008, 56, 2892–2898. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Casassa, L.F.; Keller, M.; Harbertson, J.F. Regulated Deficit Irrigation Alters Anthocyanins, Tannins and Sensory Properties of Cabernet Sauvignon Grapes and Wines. Molecules 2015, 20, 7820–7844. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. van Leeuwen, C.; Destrac-Irvine, A. Modified Grape Composition Under Climate Change: Consequences for Winemaking. OENO One 2017, 51, 147–154. [Google Scholar]
  12. Hewitt, S.; Hernández-Montes, E.; Dhingra, A.; Keller, M. Impact of Heat Stress, Water Stress, and Their Combined Effects on the Metabolism and Transcriptome of Grape Berries. Sci. Rep. 2023, 13, 9907. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Filimon, R.M.; Bunea, C.I.; Filimon, R.V.; Bora, F.D.; Damian, D. Long-Term Evolution of the Climatic Factors and Its Influence on Grape Quality in Northeastern Romania. Horticulturae 2024, 10, 705. [Google Scholar] [CrossRef] [Scilit]
  14. Rienth, M.; Lamy, F.; Schoenenberger, P.; Noll, D.; Lorenzini, F.; Viret, O.; Zufferey, V. A Vine Physiology-Based Terroir Study in the AOC-Lavaux Region in Switzerland. OENO One 2020, 54, 699–716. [Google Scholar] [CrossRef] [Scilit]
  15. Ramos, M.C.; de Toda, F.M. Variability in the Potential Effects of Climate Change on Phenology and on Grape Composition of Tempranillo in Three Zones of the Rioja DOCa (Spain). Eur. J. Agron. 2020, 115, 126014. [Google Scholar] [CrossRef] [Scilit]
  16. Meneghelli, C.M.; de Soma Lima, J.S.; Bernardes, A.L.; Coelho, J.M.; de Assis Silva, S.; Meneghelli, L.A.M. “Niágara Rosada” and “Isabel” Grapes Quality Cultivated in Different Altitudes in the State of Espírito Santo, Brazil. Emir. J. Food Agric. 2018, 30, 1014–1018. [Google Scholar]
  17. Regina, M.A.; do Carmo, E.L.; Fonseca, A.R.; Purgatto, E.; Shiga, T.M.; Lajolo, F.M.; Ribeiro, A.P.; da Mota, R.V. Altitude Influence on the Quality of “Chardonnay” and “Pinot Noir” Grapes in the State of Minas Gerais. Rev. Bras. Frutic. 2010, 32, 143–150. [Google Scholar] [CrossRef] [Scilit]
  18. VanderWeide, J.; Nasrollahiazar, E.; Schultze, S.; Sabbatini, P.; Castellarin, S.D. Impact of Cluster Thinning on Wine Grape Yield and Fruit Composition: A Review and Meta-Analysis. Aust. J. Grape Wine Res. 2024, 2024, 2504396. [Google Scholar] [CrossRef] [Scilit]
  19. Mansour, G.; Ghanem, C.; Mercenaro, L.; Nassif, N.; Hassoun, G.; Del Caro, A. Effects of Altitude on the Chemical Composition of Grapes and Wine: A Review. OENO One 2022, 56, 227–239. [Google Scholar] [CrossRef] [Scilit]
  20. Yan, H.K.; Ma, S.; Lu, X.; Zhang, C.C.; Ma, L.; Li, K.; Wei, Y.C.; Gong, M.S.; Li, S. Response of Wine Grape Quality to Rainfall, Temperature, and Soil Properties in Hexi Corridor. HortScience 2022, 57, 1593–1599. [Google Scholar] [CrossRef] [Scilit]
  21. Leolini, L.; Moriondo, M.; Romboli, Y.; Gardiman, M.S.; Costafreda-Aumedes, I.; García de Cortázar-Atauri, M.; Bindi, L.; Granchi, L.; Brilli, L. Modelling Sugar and Acid Content in Sangiovese Grapes Under Future Climates: An Italian Case Study. Clim. Res. 2019, 78, 211–224. [Google Scholar] [CrossRef] [Scilit]
  22. Gatti, M.; Garavani, A.; Cantatore, A.; Parisi, M.G.; Bobeica, N.A.; Merli, M.C.; Vercesi, A.; Poni, S. Interactions of Summer Pruning Techniques and Vine Performance in the White Vitis vinifera cv. Ortrugo. Aust. J. Grape Wine Res. 2015, 21, 80–89. [Google Scholar]
  23. Huglin, P.; Schneider, C. Biologie et Écologie de la Vigne; Tec & Doc-Lavoisier: Paris, France, 1998. [Google Scholar]
  24. Kliewer, W.M. Effect of Day Temperature and Light Intensity on Concentration of Malic and Tartaric Acids in Vitis vinifera L. Grapes. J. Am. Soc. Hortic. Sci. 1971, 96, 372–377. [Google Scholar] [CrossRef] [Scilit]
  25. Sugiura, T.; Sato, A.; Shiraishi, M.; Amamiya, H.; Ohno, H.; Takayama, N.; Miyata, N.; Sakaue, T.; Konno, S. Prediction of Acid Concentration in Wine and Table Grape Berries from Air Temperature. Hortic. J. 2020, 89, 208–215. [Google Scholar] [CrossRef] [Scilit]
  26. Barnuud, N.N.; Zerihun, A.; Mpelasoka, F.; Gibberd, M.; Bates, B. Responses of Grape Berry Anthocyanin and Titratable Acidity to the Projected Climate Change across the Western Australian Wine Regions. Int. J. Biometeorol. 2014, 58, 1279–1293. [Google Scholar] [PubMed]
  27. Vršič, S.; Vodovnik, T. Reactions of Grape Varieties to Climate Changes in North-East Slovenia. Plant Soil Environ. 2012, 58, 34–41. [Google Scholar] [CrossRef] [Scilit]
  28. Rogiers, S.Y.; Greer, D.H.; Liu, Y.; Baby, T.; Xiao, Z. Impact of Climate Change on Grape Berry Ripening: An Assessment of Adaptation Strategies for the Australian Vineyard. Front. Plant Sci. 2022, 13, 1094633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Gutiérrez-Gamboa, G.; Alañón-Sánchez, N.; Mateluna-Cuadra, R.; Verdugo-Vásquez, N. An Overview About the Impacts of Agricultural Practices on Grape Nitrogen Composition: Current Research Approaches. Food Res. Int. 2020, 136, 109477. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Baroň, M. Yeast Assimilable Nitrogen in South Moravian Grape Musts and Its Effect on Acetic Acid Production During Fermentation. Czech J. Food Sci. 2011, 29, 603–609. [Google Scholar] [CrossRef] [Scilit]
  31. Ough, C.S.; Kriel, A. Ammonia Concentrations of Musts of Different Grape Cultivars and Vineyards in the Stellenbosch Area. S. Afr. J. Enol. Vitic. 1985, 6, 7–11. [Google Scholar]
  32. Bellassai, S. Winemaking in the Era of Climate Change. Wines and Vines, Wine Business Analytics. Available online: https://winebusinessanalytics.com/features/article/201466/Winemaking-in-the-Era-of-Climate-Change (accessed on 2 April 2025).
  33. Linsenmeier, A.W.; Loos, U.; Lönhertz, O. Must Composition and Nitrogen Uptake in a Long-Term Trial as Affected by Timing of Nitrogen Fertilization in a Cool-Climate Riesling Vineyard. Am. J. Enol. Vitic. 2008, 59, 255–264. [Google Scholar] [CrossRef] [Scilit]
  34. Hilbert, G.; Soyer, J.; Molot, C.; Giraudon, J.; Milin, M.; Gaudillere, J. Effects of Nitrogen Supply on Must Quality and Anthocyanin Accumulation in Berries of cv. Merlot. Vitis 2015, 42, 69. [Google Scholar]
  35. Liu, S.-Q.; Pritchard, G.G.; Hardman, M.J.; Pilone, G.J. Arginine Catabolism in Wine Lactic Acid Bacteria: Is It via the Arginine Deiminase Pathway or the Arginase–Urease Pathway? J. Appl. Bacteriol. 1996, 81, 486–492. [Google Scholar]
  36. Hale, C.R. Interaction Between Temperature and Potassium and Grape Acids. In CSIRO Division of Horticultural Research Report; CSIRO: Burnside, Australia, 1981; pp. 87–88. [Google Scholar]
  37. Iland, P. Grape Berry Ripening: The Potassium Story. Aust. Grapegrow. Winemak. 1988, 289, 22–24. [Google Scholar]
  38. Mpelasoka, B.S.; Schachtman, D.P.; Michael, T.; Treeby, M.T.; Thomas, M.R. A Review of Potassium Nutrition in Grapevines with Special Emphasis on Berry Accumulation. Aust. J. Grape Wine Res. 2003, 9, 154–168. [Google Scholar] [CrossRef] [Scilit]
  39. Shange, L.P.; Conradie, W.J. Effects of Soil Parent Material and Climate on the Performance of Vitis vinifera L. cv. Sauvignon Blanc and Cabernet Sauvignon. Part I. Soil Analysis, Soil Water Status, Root System Characteristics, Plant Water Status, Cane Mass and Yield. S. Afr. J. Enol. Vitic. 2012, 33, 161–173. [Google Scholar]
  40. Marcuzzo, P.; Gaiotti, F.; Lucchetta, M.; Lovat, L.; Tomasi, D. Tuning Potassium Fertilization to Improve pH and Acidity in Glera Grapevine (Vitis vinifera L.) Under a Warming Climate. Appl. Sci. 2021, 11, 11869. [Google Scholar] [CrossRef] [Scilit]
  41. Duchêne, É.; Dumas, V.; Butterlin, G.; Jaegli, N.; Rustenholz, C.; Chauveau, A.; Bérard, A.; Le Paslier, M.C.; Gaillard, I.; Merdinoglu, D. Genetic Variations of Acidity in Grape Berries Are Controlled by the Interplay Between Organic Acids and Potassium. Theor. Appl. Genet. 2020, 133, 993–1008. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Martín, P.; Delgado, R.; González, M.R.; Gallegos, J.I. Colour of Tempranillo Grapes as Affected by Different Nitrogen and Potassium Fertilization Rates. Acta Hortic. 2004, 652, 153–160. [Google Scholar] [CrossRef] [Scilit]
  43. Poni, R.; Quartieri, M.; Taliavini, M. Potassium Nutrition of Cabernet Sauvignon Grapevines (Vitis vinifera L.) as Affected by Shoot Trimming. Plant Soil 2003, 253, 341–351. [Google Scholar] [CrossRef] [Scilit]
  44. Garcia, M.; Gallego, P.; Daverède, C.; Ibrahim, H. Effect of Three Rootstocks on Grapevine (Vitis vinifera L.) cv. Négrette, Grown Hydroponically. Potassium, Calcium and Magnesium Nutrition. S. Afr. J. Enol. Vitic. 2001, 22, 101–103. [Google Scholar]
  45. Nistor, E.; Dobrei, A.G.; Mattii, G.B.; Dobrei, A. Calcium and Potassium Accumulation During the Growing Season in Cabernet Sauvignon and Merlot Grape Varieties. Plants 2022, 11, 1536. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Agenbach, G. Experiments to Modify Grape Juice Potassium Content and Wine Quality on Granite Derived Soils near Paardeberg. Master’s Thesis, Stellenbosch University, Stellenbosch, South Africa, 2006. [Google Scholar]
  47. Esteban, M.A.; Villanueva, M.J.; Lisaarrague, J.R. Effect of Irrigation on Changes in Berry Composition of Tempranillo During Maturation. Sugars, Organic Acids, and Mineral Elements. Am. J. Enol. Vitic. 1999, 50, 418–434. [Google Scholar] [CrossRef] [Scilit]
  48. Smart, R.E. Principles of Grapevine Canopy Microclimate Manipulation with Implications for Yield and Quality. A Review. Am. J. Enol. Vitic. 1985, 36, 230–239. [Google Scholar] [CrossRef] [Scilit]
  49. Watrelot, A.A.; Norton, E.L. Chemistry and Reactivity of Tannins in Vitis spp.: A Review. Molecules 2020, 25, 2110. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Ribéreau-Gayon, P.; Glories, Y.; Maujean, A.; Du Bourdieu, D. Handbook of Enology: The Chemistry of Wine Stabilisation and Treatment, 2nd ed.; John Wiley & Sons Inc.: New York, NY, USA, 2006. [Google Scholar]
  51. Tarara, J.M.; Lee, J.; Spayd, S.E.; Seagal, C.F. Berry Temperature and Solar Radiation Alter Acylation, Proportion and Concentration of Anthocyanin in Merlot Grapes. Am. J. Enol. Vitic. 2008, 59, 235–247. [Google Scholar] [CrossRef] [Scilit]
  52. Bindon, K.; Pendleton, P.; Smith, P.; Kennedy, J. Factors Affecting Skin Tannin Extractability in Ripening Grapes. J. Agric. Food Chem. 2014, 62, 1130–1141. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  53. Downey, M.O.; Dokoozlian, N.K.; Krstic, M.P. Cultural Practice and Environmental Impacts on the Flavonoid Composition of Grapes and Wine: A Review on Recent Research. Am. J. Enol. Vitic. 2006, 57, 257–268. [Google Scholar] [CrossRef] [Scilit]
  54. Gouot, J.C.; Smith, J.P.; Holzapfel, B.P.; Walker, A.R.; Barril, C. Grape Berry Flavonoids: A Review of Their Biochemical Responses to High and Extreme High Temperatures. J. Exp. Bot. 2019, 70, 397–423. [Google Scholar] [PubMed]
  55. Fournand, D.; Vicens, A.; Sidhoum, L.; Souquet, J.-M.; Moutounet, M.; Cheynier, V. Accumulation and Extractability of Grape Skin Tannins and Anthocyanins at Different Advanced Physiological Stages. J. Agric. Food Chem. 2006, 54, 7331–7338. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  56. Bene, Z. Impact of Climate Change on the (Poly)phenol Composition of Botrytization in the Tokaj Wine Region. J. Nutr. Food Process. 2024, 7, 11. [Google Scholar] [CrossRef] [Scilit]
  57. Cataldo, E.; Eichmeier, A.; Mattii, G.B. Effects of Global Warming on Grapevine Berries Phenolic Compounds—A Review. Agronomy 2023, 13, 2192. [Google Scholar] [CrossRef] [Scilit]
  58. Barreto de Oliveira, J.; Egipto, R.; Laureano, O.; de Castro, R.; Pereira, G.E.; Ricardo-da-Silva, J.M. Climate Effects on Physicochemical Composition of Syrah Grapes at Low and High Altitude Sites from Tropical Grown Regions of Brazil. Food Res. Int. 2019, 121, 870–879. [Google Scholar] [CrossRef] [Scilit]
  59. Koblet, W.; Zanier, C.; Tanner, H.; Vautier, P.; Simon, J.-L.; Gnägi, F. Reifeverlauf von Sonnen- und Schattentrauben. Schweiz. Z. Obst-Weinbau 1977, 113, 558–567. [Google Scholar]
  60. McMaster, G.S.; Wilhelm, W.W. Growing Degree-Days: One Equation, Two Interpretations. Agric. For. Meteorol. 1997, 87, 291–300. [Google Scholar] [CrossRef] [Scilit]
  61. Quinn, F.H.; Assel, R.A.; Boyce, D.E.; Lèskevich, G.A.; Snider, C.R.; Weisnet, D. Summary of Great Lakes Weather and Ice Conditions, Winter 1976–77; NOAA Technical Memorandum ERL GLERL-20; Great Lakes Environmental Research Laboratory: Ann Arbor, MI, USA, 1978. [Google Scholar]
  62. Gladstones, J. Viticulture and Environment; Winetitles: Adelaide, Australia, 1992. [Google Scholar]
  63. Gladstones, J. Past and Future Climatic Indices for Viticulture. In Proceedings of the 5th International Symposium for Cool Climate Viticulture and Oenology, Melbourne, Australia, 16–20 January 2000. [Google Scholar]
  64. Huglin, P. Nouveau Mode d’Évaluation des Possibilités Héliothermiques d’un Milieu Viticole. C. R. Acad. Agric. Fr. 1978, 64, 1117–1126. [Google Scholar]
  65. Amerine, M.A.; Winkler, A.J. Composition and Quality of Musts and Wines of California Grapes. Hilgardia 1944, 15, 493–675. [Google Scholar] [CrossRef] [Scilit]
  66. Winkler, A.J.; Cook, J.A.; Kliere, W.M.; Lider, L.A. General Viticulture, 2nd ed.; University of California Press: Berkeley, CA, USA, 1974. [Google Scholar]
  67. Tonietto, J.; Carbonneau, A. A Multicriteria Climatic Classification System for Grape Growing Regions Worldwide. Agric. For. Meteorol. 2004, 124, 81–97. [Google Scholar] [CrossRef] [Scilit]
  68. Jones, G.V.; Goodrich, G.B. Influence of Climate Variability on Wine Region in the Western USA and on Wine Quality in the Napa Valley. Clim. Res. 2008, 35, 241–254. [Google Scholar] [CrossRef] [Scilit]
  69. Happ, E. Indices for Exploring the Relationship Between Temperature and Grape and Wine Flavour. Aust. N. Z. Wine Ind. J. 1999, 14, 68–75. [Google Scholar]
  70. Dry, P.; Smart, R.E. The Grape Growing Regions of Australia. In Viticulture Volume. 1 Resources; Coombe, B.G., Ed.; Winetitles: Adelaide, Australia, 1988; Volume 1. [Google Scholar]
  71. Katz, R.W. Statistical Procedures for Making Inferences About Climate Variability. J. Clim. 1988, 1, 1057–1064. [Google Scholar] [CrossRef] [Scilit]
  72. Sabatelli, M.P.; Stendardi, M.L. Influence of Some Meteorological Factors During the First Months of the Vegetative Cycle on the Sugar Content in the Berries of Some Grape cvs. Riv. Vitic. Enol. 1981, 34, 271–276. [Google Scholar]
  73. Salinari, F.; Giosuè, S.; Tubiello, F.N.; Rettori, A.; Rossi, V.; Spanna, F.; Rosenzweig, C.; Gullino, M.L. Downy Mildew (Plasmopara viticola) Epidemics on Grapevine Under Climate Change. Glob. Change Biol. 2006, 12, 1299–1307. [Google Scholar] [CrossRef] [Scilit]
  74. Nicholas, P.; Magarey, P.; Wachtel, M. Diseases and Pests. In Grape Production Series; Winetitles: Adelaide, Australia, 1994; p. 106. [Google Scholar]
  75. Allen Consulting Group. Climate Change, Risk and Vulnerability. Promoting an Efficient Adaptation Response in Australia; Final Report; Australian Greenhouse Office: Canberra, Australia, 2005. [Google Scholar]
  76. Ribéreau-Gayon, P.; Guimberteau, G. Vintage Reports: 1988–1996; University of Bordeaux: Bordeaux, France, 1996. [Google Scholar]
  77. Dunkel, Z.; Kozma, F.; Major, G. Szőlőültetvényeink Hőmérséklet- és Sugárzásellátottsága a Vegetációs Időszakban. Időjárás 1981, 85, 226–234. [Google Scholar]
Figure 1. Geographical layout of the study site (Tokaj wine region, NE Hungary). Geolocation of the monitoring stations: Szent Tamás L (N48.189603, E21.297463), Szilvás (N48.187303, E21.308468), Betsek L (N48.183508, E21.316703), Betsek U (N48.187240, E21.318381), Szent Tamás U (N48.191026, E21.293183), Kővágó (N48.195164, E21.308718). Vineyards are marked in green contouring. Main map scale: 1:40,000. Note: Labels on the map (e.g., Mád) indicate the official names of the Hungarian municipalities and specific vineyard locations within the Tokaj Wine Region where the experimental monitoring stations were established.
Agronomy 16 01253 g001
Figure 2. Phenological distribution of key climatic parameters during the 2022–2024 growing seasons. Data represent the average of six monitoring locations. (a) Precipitation and thermal accumulation profile: Bubble centers are positioned at the midpoint of each phenological stage with their Y coordinates corresponding to the cumulative growing degree days (GDD, (°C d). Bubble size is proportional to global solar irradiation (kJ m−2 day−1). Bubble body color and frame color represent anomalies in rainfall depth and the number of rainy days, respectively. Values are expressed on a six-point scale (see color key in chart) as relative deviations from the long-term mean (2002–2024, Tarcal, HungaroMet). (b) Thermal dynamics and stage duration: Horizontal bars indicate stage-specific mean temperatures (°C), with the duration (days) displayed in circles at the stage midpoints. Vertical spikes represent daily maximum and minimum temperatures. Abbreviations: BB: bud burst; FW: flowering; BPS: berries pea-size; VRS: véraison; PVR: post-véraison; BS: berry sampling; LF: leaf fall (e.g., BB–FW indicates the period from bud burst to flowering).
Agronomy 16 01253 g002
Table 1. Impact of the vintage (2022–2024) on must quality represented as pooled regional means based on non-parametric testing.
(Mean ± Std. Error) 202220232024
Total titratable acidity (TTA) **g L−16.30 ± 0.76 a6.25 ± 0.48 a3.63 ± 0.45 b
pH **-3.17 ± 0.07 a3.28 ± 0.05 ab3.61 ± 0.12 b
Ammonium (NH4+)mg L−145 ± 13 a55 ± 16 a60 ± 16 a
Potassium (K+) *mg L−11095 ± 118 ab1266 ± 181 a882 ± 242 b
Tannic acidTAEg L−10.23 ± 0.06 a0.31 ± 0.06 a0.26 ± 0.05 a
Sampling included 200–250 berries from five vines per site (six stations across the studied vineyards, n = 30 annually). Significance levels: α = 0.05 * and α = 0.01 **. Parameters marked with different letters show significant year-to-year variation. (Graphical representations are available as boxplots in Appendix C, Figure A1).
Table 2. Statistical analysis of primary candidate climatic correlates and their associations with total titratable acidity (2022–2024).
ParameterPeriodANOVATests of NormalityCorrelation Coefficients
Kruskal–Wallis H TestKolmogorov–Smirnov TestShapiro–Wilk TestSpearmanPearsonR2
ERDJUL0.00020.00000.0000−0.82 0.67
NTNBPS-VRS0.00340.05750.1569 −0.820.67
NSDVRS-PVR0.00030.00000.0000−0.81 0.65
BEDDBB-FW0.00050.02320.00550.80 0.64
AVG TMAXFW-BPS0.00080.00030.00070.80 0.64
GDDBB-FW0.00050.02730.00570.80 0.63
MIN TAVGPVR-BS0.00170.00000.00010.79 0.62
HRDAUG0.00370.00000.0000−0.77 0.60
MIN TMAXBB-FW0.00050.02670.00980.75 0.56
MIN TMAXPVR-BS0.00150.02280.00470.74 0.55
AVG TAVGFW-BPS0.00050.00000.00020.74 0.55
HRDJUL0.00040.00000.0012−0.74 0.55
HRDJUN0.00030.00080.0010−0.73 0.54
NSDFW-BPS0.00070.03710.04960.73 0.54
NTNPVR-BS0.00050.00050.0020−0.70 0.49
Parameter abbreviations are defined in Table A3 (Appendix B). BB-FW: bud burst to flowering; FW-BPS: flowering to berries pea-size; BPS-VRS: berries pea-size to véraison; VRS-PVR: véraison to post-véraison; PVR-BS: post-véraison to berry sampling; JUN, JUL, AUG: calendar months. Correlation analysis is based on the pooled regional data from the six microclimatic monitoring stations. Note: All listed parameters and coefficients are statistically significant (p ≤ 0.05) due to the prior multi-step screening protocol.
Table 3. Statistical analysis of primary candidate climatic correlates and their associations with pH (2022–2024), derived from the pooled regional monitoring network.
ParameterPeriodANOVATests of NormalityCorrelation Coefficients
Kruskal–Wallis H TestKolmogorov–Smirnov TestShapiro–Wilk TestSpearmanPearsonR2
NEHDBB-BS0.00060.01260.0009−0.94 0.87
BEDDBB-FW0.00050.02320.0055−0.93 0.87
GDDBB-FW0.00050.02730.0057−0.93 0.87
HRDJUN0.00030.00080.00100.93 0.86
AVG TMAXFW-BPS0.00080.00030.0007−0.93 0.86
MAX TMAXBB-BS0.00050.20000.3818 −0.910.83
IRPVR-BS0.00150.00000.00010.91 0.83
MIN TMAXBB-FW0.00050.02670.0098−0.91 0.83
HRDSFBB-BS0.00060.08270.0571 0.910.83
NHDFW-BPS0.00070.00070.0004−0.91 0.82
NSDFW-BPS0.00070.03710.0496−0.90 0.82
GDDVRS-PVR0.00050.20000.0834 0.900.81
MAX TMAXBB-FW0.00050.20000.2126 −0.900.80
AVG TAVGFW-BPS0.00050.00000.0002−0.88 0.77
ERDJUN0.00030.02220.00580.87 0.76
MIN TAVGPVR-BS0.00170.00000.0001−0.87 0.76
AVG TMAXBB-FW0.00050.20000.0643 −0.870.76
ERDSFBB-BS0.00030.00030.00410.87 0.76
BEDDVRS-PVR0.00040.00030.00040.87 0.75
RainfallJUN0.00050.02770.00590.86 0.75
BEDDPVR-BS0.00050.00000.00010.86 0.74
Parameter abbreviations are defined in Table A3 (Appendix B). BB-FW: bud burst to flowering; FW-BPS: flowering to berries pea-size; VRS-PVR: véraison to post-véraison; PVR-BS: post-véraison to berry sampling; BB-BS: bud burst to berry sampling; SFBB-BS: bud burst (based on sap flow activity) to berry sampling; JUN: June. Correlation analysis is based on the pooled regional data from the six microclimatic monitoring stations. Note: All listed parameters and coefficients are statistically significant (p ≤ 0.05) due to the prior multi-step screening protocol.
Table 4. Statistical analysis of candidate climatic correlates and their associations with ammonia content (2022–2024).
ParameterPeriodANOVATests of NormalityCorrelation Coefficients
Kruskal–Wallis H TestKolmogorov–Smirnov TestShapiro–Wilk TestSpearmanPearsonR2
MAX TMINMAY0.02220.16510.0887 0.690.48
HRDMAY0.00920.00140.00290.62 0.38
HRDFW-BPS0.00150.00000.00010.56 0.31
MIN TAVGBPS-VRS0.00340.01800.02350.53 0.28
BEDDBPS-VRS0.00050.00290.00060.52 0.27
RDSFBB-BS0.00160.00000.00010.47 0.22
NHDFW-BPS0.00070.00070.0004−0.46 0.21
NSDPVR-BS0.00120.00000.00010.46 0.21
NSDBPS-VRS0.00070.00860.00260.46 0.21
RainfallMAY0.00060.15460.1386 0.450.20
IRPVR-BS0.00150.00000.00010.45 0.20
Parameter abbreviations are defined in Table A3 (Appendix B). FW-BPS: flowering to berries pea-size; BPS-VRS: berries pea-size to véraison; BS: post-véraison to berry sampling; SFBB-BS: bud burst (based on sap flow activity) to berry sampling; MAY: calendar month. Correlation analysis is based on the pooled regional data from the six microclimatic monitoring stations. Note: All listed parameters and coefficients are statistically significant (p ≤ 0.05) due to the prior multi-step screening protocol.
Table 5. Statistical analysis of candidate climatic correlates and their associations with potassium content (2022–2024).
ParameterPeriodANOVATests of NormalityCorrelation Coefficients
Kruskal–Wallis H TestKolmogorov–Smirnov TestShapiro–Wilk TestSpearmanPearsonR2
NTNVRS-PVR0.01470.20000.1970 0.830.68
MIN TAVGMAY0.00270.00050.0011−0.82 0.68
MAX TAVGVRS-PVR0.00060.20000.3003 0.780.61
NHDSFBB-BS0.00260.08850.0622 −0.760.58
NSDJUL0.00080.00010.0039−0.76 0.57
MIN TAVGBPS-VRS0.00340.01800.0235−0.73 0.53
NHDAUG0.00250.20000.4015 −0.720.52
RDJUL0.00050.02480.01490.72 0.51
AVG TMAXAUG0.00460.20000.6615 −0.700.48
GDDBB-BS0.00050.20000.1346 −0.680.47
NSDVRS-PVR0.00030.00000.0000−0.67 0.45
Parameter abbreviations are defined in Table A3 (Appendix B). BPS-VRS: berries pea-size to véraison; VRS-PVR: véraison to post-véraison; BB-BS: bud burst to berry sampling; SFBB-BS: bud burst (based on sap flow activity) to berry sampling; MAY, JUL, AUG: calendar months. Correlation analysis is based on the pooled regional data from the six microclimatic monitoring stations. Note: All listed parameters and coefficients are statistically significant (p ≤ 0.05) due to the prior multi-step screening protocol.
Table 6. Statistical analysis of primary candidate climatic correlates and their associations with tannic acid content (2022–2024).
ParameterPeriodANOVATests of NormalityCorrelation Coefficients
Kruskal–Wallis H TestKolmogorov–Smirnov TestShapiro–Wilk TestSpearmanPearsonR2
MAX TMAXJUN0.00170.02270.0391−0.77 0.60
MAX TMAXMAY0.00130.00170.0044−0.76 0.58
AVG TMAXPVR-BS0.00270.20000.6539 −0.730.54
AVG TMAXBB-BS0.00310.00350.0174−0.73 0.53
MAX TAVGJUN0.00050.00370.0019−0.73 0.53
AVG TMAXBPS-VRS0.00280.08930.1428 −0.710.51
BEDDBLP0.00120.20000.8993 −0.710.50
GDDBLP0.00190.00680.0123−0.71 0.50
MIN TMAXVRS-PVR0.00190.20000.1710 −0.710.50
IRDAVGBPS-VRS0.00050.20000.3492 −0.690.47
MAX TAVGFW-BPS0.00050.00200.0011−0.68 0.46
MIN TMAXFW-BPS0.00050.00100.0015−0.67 0.44
MIN TAVGFW-BPS0.00050.00570.0026−0.66 0.44
BEDDAUG0.00040.00000.0001−0.65 0.43
DRTBB-FW0.02410.20000.3634 −0.640.41
NHDSFBB-BS0.00260.08850.0622 −0.640.41
DRTJUN0.01450.20000.9207 −0.620.39
IRMAY0.00230.20000.1594 −0.610.37
IRDAVGMAY0.00230.20000.1594 −0.610.37
MIN TAVGVRS-PVR0.00050.03470.0091 −0.580.34
Parameter abbreviations are defined in Table A3 (Appendix B). BB-FW: bud burst to flowering; FW-BPS: flowering to berries pea-size; BPS-VRS: berries pea-size to véraison; VRS-PVR: véraison to post-véraison; PVR-BS: post-véraison to berry sampling; BB-BS: bud burst to berry sampling; SFBB-BS: bud burst (based on sap flow activity) to berry sampling; BLP: blooming period (15 May–15 June); MAY, JUN, AUG: calendar months. Correlation analysis is based on the pooled regional data from the six microclimatic monitoring stations. Note: All listed parameters and coefficients are statistically significant (p ≤ 0.05) due to the prior multi-step screening protocol.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.