


Abstract
This paper aimed to study the adaptation of a crop to the specific climatic conditions of southern Romania, Pitești-Mărăcineni, Romania, in terms of the phenology of two chokeberry (Aronia melanocarpa) cultivars (‘Melrom’ and ‘Nero’). The BBCH (Biologische Bundesantalt, Bundessortenamt and Chemische Industrie) scale was used for phenological observations. The recorded data were statistically processed, calculating the average onset time and duration of fruiting phenophases and dormancy duration, average air temperatures, total solar radiation, and the cold and heat accumulation. Bud swelling was registered between 28 January and 8 February, budburst occurred starting on 3 March, while flowering began in stages, between 15 April and 1 May, and was completed between 27 April and 14 May. During the 154 days of 53–87 BBCH, the average air temperature, 16.1 °C, ranged between the extremes of −6.1 and 36.8 °C. The onset data and spring–summer phenophases were mainly related to the minimum air-temperature oscillations. The flowering timing shortened as the maximum temperature and total solar radiation increased. The relation between the environmental factors and the flowering strategy indicates the A. melanocarpa as a species adapted to the temperate continental climate of southern Romania.
1. Introduction
Climate change’s impact on plants is an ever-growing research challenge that scientists in plant biology and agricultural sciences need to address in this period. In the present study, the authors selected chokeberry as the object of study. Chokeberry (Aronia melanocarpa) is a deciduous shrub native to eastern North America and Canada, whose cultivation spread to Europe after the 19th century [1,2], due mainly to the interest in its antioxidant compounds [3]. Chokeberry is a deciduous shrub belonging to the Rosaceae family. The fruit is edible, although very astringent, and is produced from five to six bunches of flowers that bloom in late spring. Chokeberry has proven to be a species with a superior ability to adapt to pedoclimatic conditions (such as wet habitats, but also dunes, rocky slopes and steep cliffs, and on over-grown or bare rocky outcrops). In addition, chokeberry crops need a low nutrient supply [4], succeeding even in the absence of fertilizer administration. This was proven by studies on the chokeberry spreading, like an invasive plant, in spontaneous flora [5,6]. It tolerates arid or excessively moist soils [4] and very low temperatures, and is also resistant to diseases and pests [7]. These features enable the cultivation of chokeberry with fewer phytosanitary treatments, as well as for the rehabilitation by populating with the vegetation of lands abandoned after the extraction of peat [4].
The success of a species depends mainly on pedoclimatic conditions and its ability to develop strategies for adapting to a constantly changing environment. Temperature, soil moisture, available nitrogen levels, light, and high levels of carbon dioxide variations affect plant phenology. Among the environmental factors, temperature plays a predominant role in controlling the proper growth and flowering of plants [8,9,10,11,12]. Most of plants require a “hot-cold-hot” sequence to complete their annual cycle [13]. Lack of exposure to low temperatures leads to slow growth of shoots in spring and severe flowering disorders, with consequences on fruit production [14,15]. The timing of phenological events, such as the appearance of leaves and flowering, strongly influences the survival of plants and is closely dependent on the evolution of environmental factors [16]. Their study is vital to understanding how plants will respond to climate change. Moreover, advancing our understanding of the triggers of phenological responses may provide insight into future states of species distribution [17,18]. Eastern Europe has a temperate continental climate, but following the global warming trend is, at the same time, experiencing increasing climatic accidents [19]. In many cases, plant growth and development (especially the quantity and quality of the fruit crop) are mainly determined by the extreme climatic phenomena that impact the physiological processes that are running during that moment. Plant phenology—the timing of plant life-cycle events, such as flowering or leafing out—plays a fundamental role in the functioning of terrestrial ecosystems, including human agricultural systems [20]. Variations in plant phenology also influence the organisms that depend on them in terrestrial ecosystems and, vice versa, the gaps between the phenology of plants and their pollinators have repercussions on crop productivity [21]. Moreover, changes in the timing of plant development sequences can expose plants not only to climatic accidents but also to diseases [22] and pest attacks [23]. In addition, one of the main strategies of sustainable agriculture is the efficient management of cultural practices, which can be accomplished by the use of well-adapted species and cultivars.
Given these aspects, in the context of global climate change, research concerning the suitable adaptation of temperate fruit crops in different crop areas is needed. This paper aimed to study the adaptation of a crop to the specific environmental conditions of southern Romania, Pitești-Mărăcineni, Romania, in terms of the phenology of two chokeberry (Aronia melanocarpa) cultivars (‘Melrom’ and ‘Nero’).
2. Materials and Methods
2.1. Material and Study Area
The vegetal material was represented by two chokeberry (Aronia melanocarpa) cultivars (‘Melrom’ and ‘Nero’), planted on individual plots, at the Research Institute for Fruit Growing Pitesti—Maracineni (E44°54′11″ N 24°52′29″ E, 287 m elevation a.s.l.) in 2011 (‘Nero’) and 2017 (‘Melrom’). The plants, obtained through micropropagation, were managed as a bush, with planting distances of 1.4 × 3.0 m (2380 plants/ha). In Romania, chokeberry has been cultivated since 1986 and is represented mostly through the ‘Nero’ and ‘Melrom’ cultivars. The phenological observations were made over three seasons of vegetation, from 2019 to 2021, on three groups of 10 mature shrubs for each cultivar, randomly chosen. The experimental chokeberry plots are located on a meadow terrace of Arges River. As Chitu [24] mentioned, according to the Köppen-Geiger classification, the Pitești-Mărăcineni area is characterized by a humid continental climate, Cfbx category. The multiannual average temperature (1969–2019) of the air was 9.9 °C, and the sum of precipitation was 680 mm. As described by Nicola et al. [25], the soil belongs to the class of wet phreatic aluviosol protisols, formed on fluvial deposits, with a loam-sandy granulometric composition. It is characterized by a strongly moderate acid reaction, a low humus content, and a low assimilable phosphorus content in the arable layer. No fertilizer or irrigation was applied.
2.2. Methods
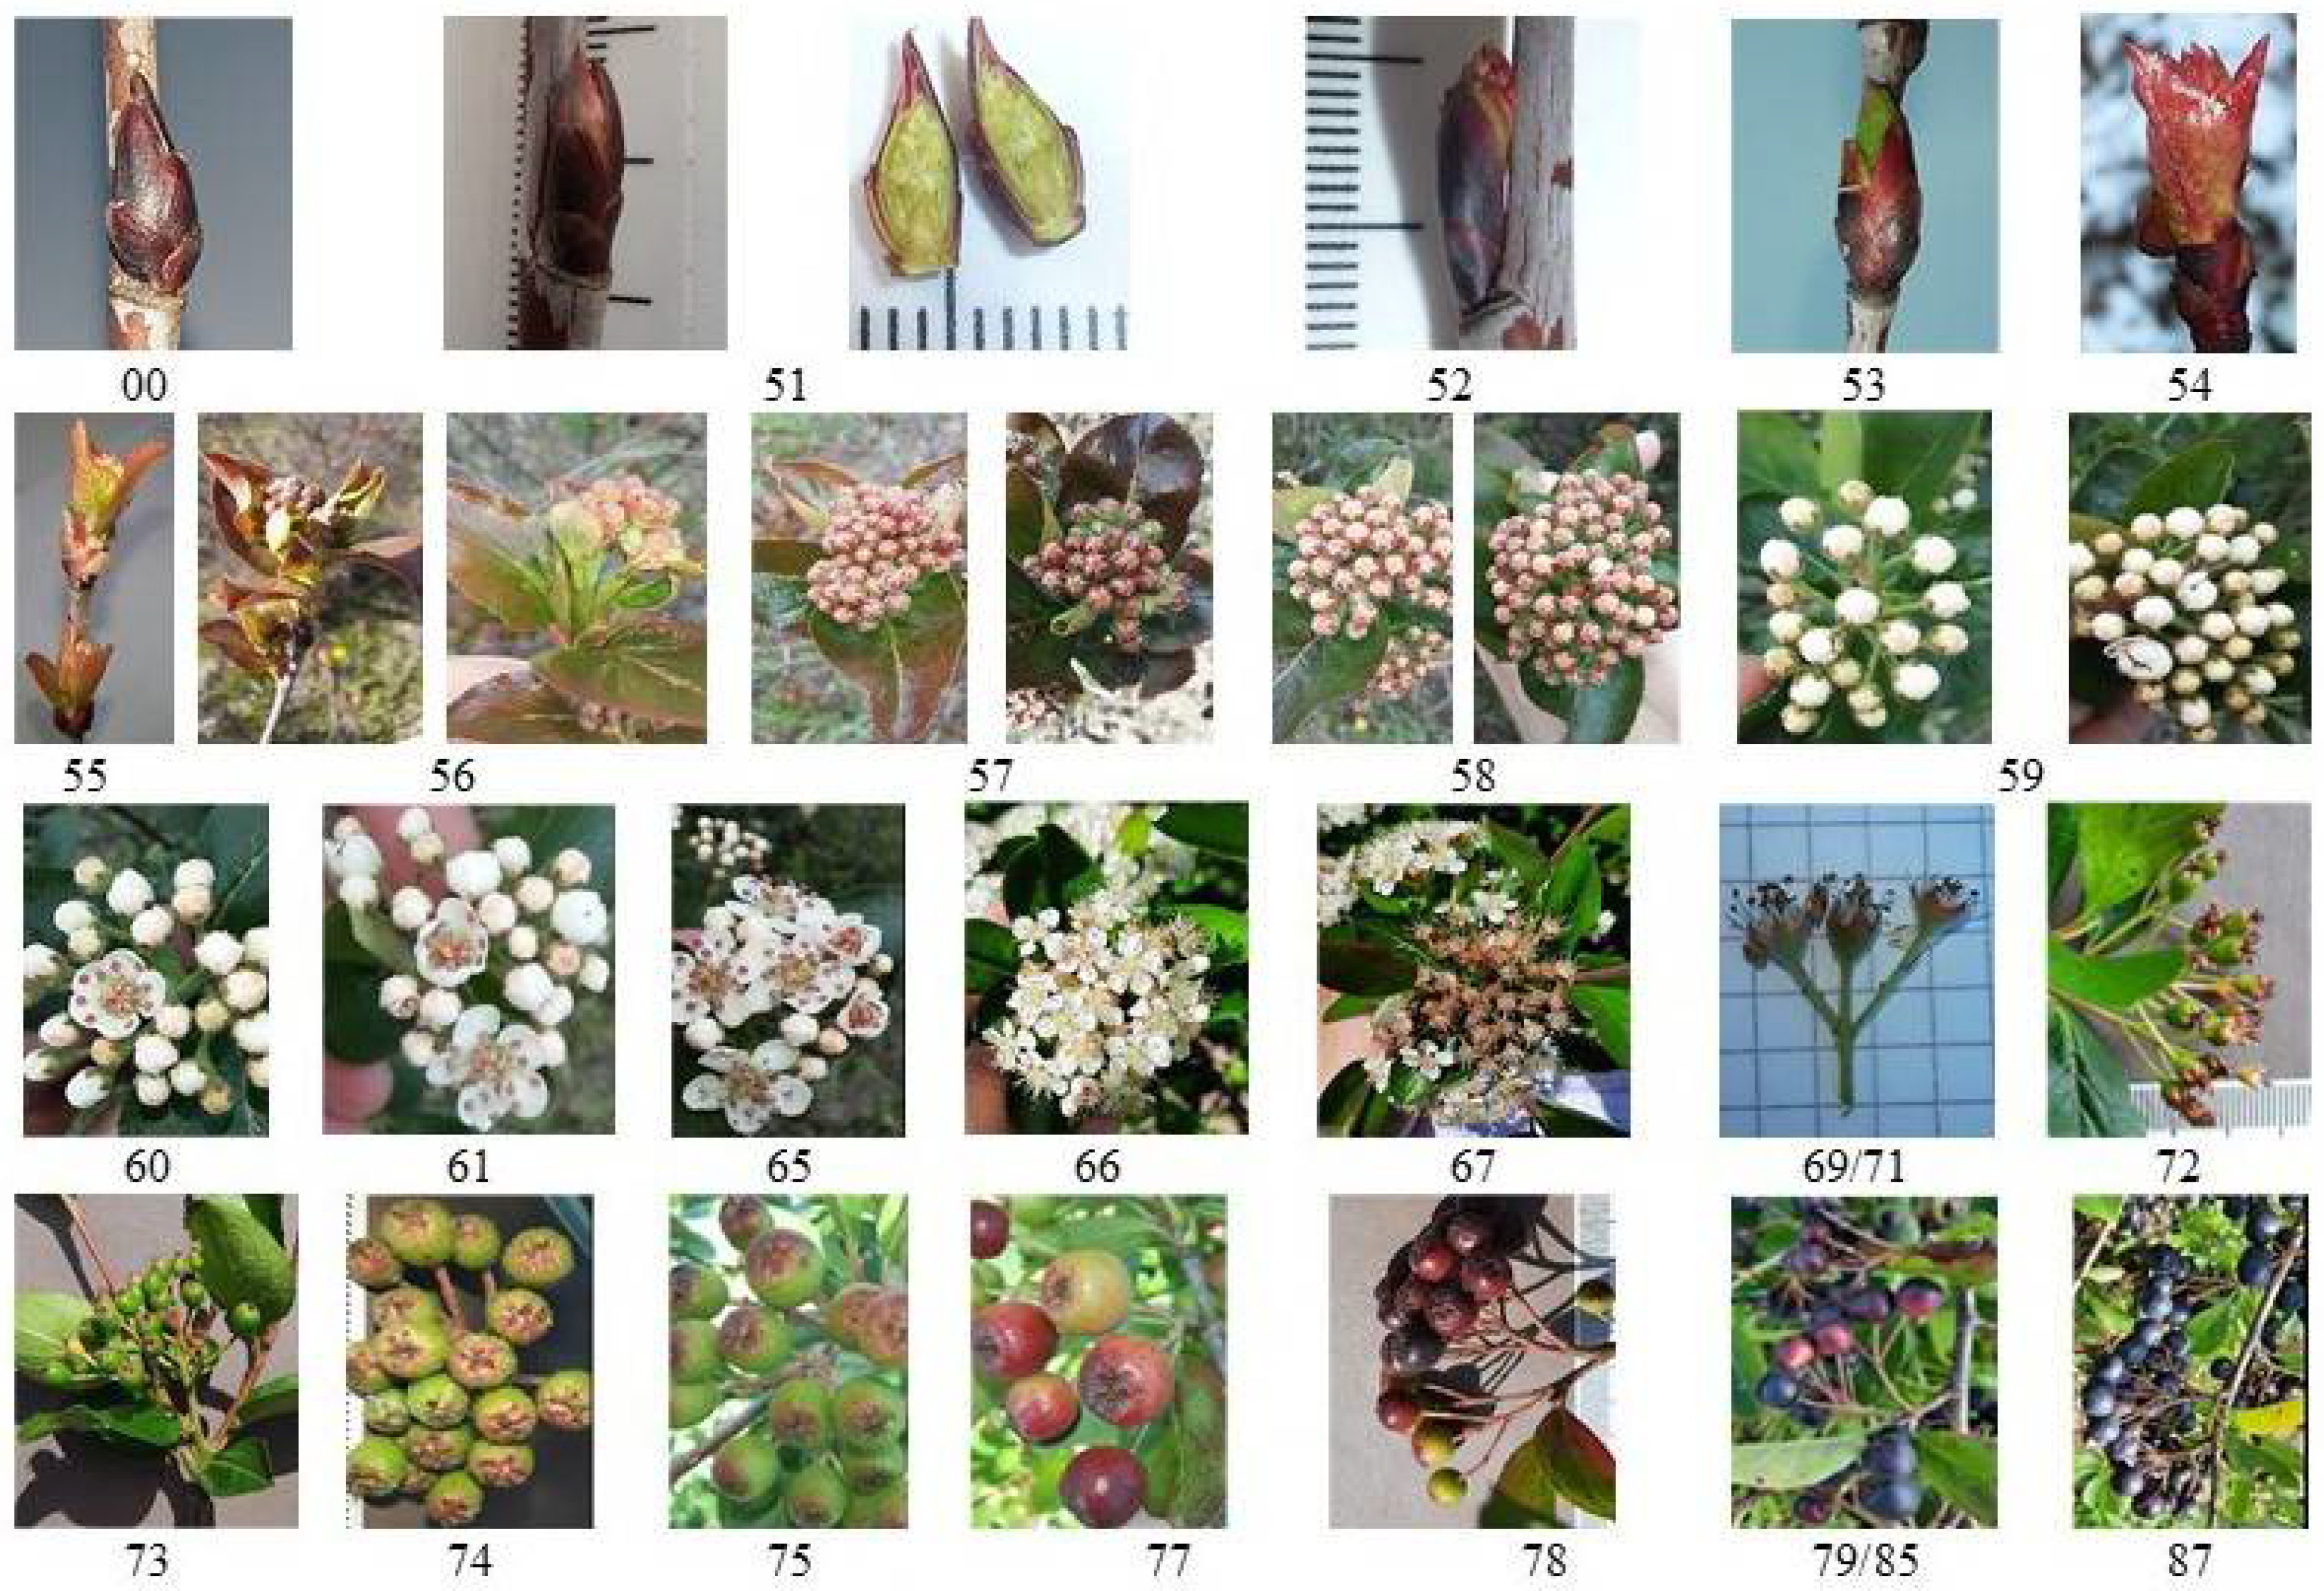
Phenological observations were performed weekly or every 2–3 days, using the BBCH scale (Figure 1) [26]. The registered data were statistically processed to calculate the length, using the number of days from 1 November and 1 January to the landmark stage.
Figure 1.
Phenophases of A. melonocarpa species in southern Romania, Pitești-Mărăcineni, Romania (00 = dormancy, 51 = inflorescence buds swelling, 52 = end of bud swelling, 53 = bud burst, 54 = mouse-ear stage, 55 = flower buds visible, 56 = single flowers separating, 57 = pink bud stage, 59 = most flowers with petals forming a hollow ball, 60 = first flowers open, 61= beginning of flowering, 65 = full flowering, 67 = flowers fading, 71 = fruit size up to 3 mm, 74 = fruit diameter up to 40 mm, 75 = fruit about the half final size, 77 = fruit about 70% final size, 78 = fruit about 80% final size, 79 = fruit about 90% final size, 85 = advanced ripening, 87 = fruit ripe for picking).
The monthly evolution, in the 49 years that preceded the present experiment (1969–2017), in average air temperatures, absolute maximums, and minimums in the area where the research was conducted were taken as a reference to present the climatic data that described the three experimental years. Data for climate analysis were collected from the automated weather station, WhatchDog900ET (Spectrum Technologies Inc., Aurora, IL, USA), located in the vicinity of the two experimental lots. The following data were recorded: air temperature (collected in the meteorological shelter, at 2 m above ground level) and the minimum temperature measured outside the meteorological shelter (shielded from direct solar radiation). Based on these data, the average temperature and the average values of the minimum and maximum temperatures recorded daily, were calculated. Average total solar radiation (W/m2) was calculated starting from daily mean values measured using WatchDog 2900ET sensor (Spectrum Technologies Inc., USA). The (current) heat accumulation (ADD = actual degree days) for the analyzed phenophases was automatically calculated by the weather station’s integrated program, by summing the determinations made every 10 min, between the initial moment, i = 0, and the final moment, t, based on Formula (1).
where, if Tmax is above the upper limit (30 °C), it will be considered that Tmax = 30 °C, and if Tmin has a value below the basal temperature (5 °C), it will be considered that Tmin = Tbasal. Temperatures of 5 and 30 °C, respectively, were considered as the absolute minimum and maximum temperatures of A. melanocarpa species based on similarities with another species of fruit bush, Ribes nigrum [27]. To calculate the cold requirement (CH = Chill Hours, it was applied chill hours), the model originally proposed by Weinberger was applied [28], which has been mentioned quite frequently by other researchers [29,30,31,32]. This model calculates the chill demand at a moment, t (CHt), after a fixed start time is given, by summing up the hours when the temperature is below 7.22 °C and above 0 °C, according to Formula (2).
where, if H is in the range 0.00–7.22 °C, H receives the value 1, and outside the domain 0.00–7.22 °C, it receives the value 0.
The chill requirement was calculated from the moment the plants started dormancy (arbitrary chosen as 1 November) and from 1 January, until bud swelling.
2.3. Data Analysis
The IBM SPSS Statistics 28 software platform was used to calculate the descriptive statistical indicators, the study of the cultivar influence (analysis of variance ANOVA), and the correlations between climatic parameters and phenophase duration, as well as between phenophase length.
3. Results and Discussion
Reproductive processes, including the timing and duration of flowering, as well as fruiting, may determine the limits of species distribution [33] and may influence annual net production [34]. The optimal flowering time of a plant, one of the variables that condition the pollination process, is determined by genetic factors, biotic interactions, and abiotic environmental variables [10,13,35,36]. The results regarding the influence of environmental factors on the chokeberry phenology are presented in Table 1, Table 2, Table 3, Table 4 and Table 5. Regarding the study area, compared to the multiannual average values, the study period was mostly characterized by higher average temperatures (Table 1). The absolute maximum values over the three years of study were below the multiannual values, except for February 2021, when the absolute maximum exceeded the multiannual values by 0.9 °C. In addition, the absolute minimum values did not fall below the normal values (−24 °C). The average monthly temperatures generally exceeded the multiannual values, especially over June–August, although the absolute daily maximum values over those three months did not exceed the normal values.
Table 1.
Temperature, sunshine hours and rainfall during 2018–2021, compared to multiannual values (1969–2017) (Pitești-Mărăcineni area).
Table 2.
Air temperature, total solar radiation (TSR), cold accumulation (CH), heat accumulation (ADD) and timing of phenophases in chokeberry (1 November 2018–20 August 2021) a.
Table 3.
Correlations between chokeberry spring–summer phenology (onset and duration) and climatic parameters (air temperature, total solar radiation) (Pitești-Mărăcineni, 2018–2021) a.
Table 4.
Correlations between chokeberry spring–summer phenophases onset and duration (Pitești-Mărăcineni, 2018–2021) a.
Table 5.
Correlations between chokeberry phenology and preceding climatic parameters (air temperatures, total solar radiation) (Pitești-Mărăcineni, 2018–2021) a.
The spring–summer phenology (inflorescence emergence, flowering, fruit development, and maturity of fruit and seed) of the chokeberry species (cultivars ‘Melrom’ and ‘Nero’) did not indicate significant differences between the studied cultivars. Table 2 shows the average data on phenophases’ development in the chokeberry. The 1 November—inflorescence buds swelling (BBCH 51) period covered an average of 94.2 ± 3.9 days (CV = 4.1%). The dormancy (1 November to 51 BBCH) ended between 28 January (2020, ‘Melrom’ and ‘Nero’) and February 8 (2021, ‘Melrom’) and occurred at air temperatures oscillating between the extremes of −14.1 and 21.4 °C, while the average of the minimum daily temperatures (Tmin) varied between −2.6 and −0.5 °C, and the average of the maximum daily temperatures (Tmax) oscillated from 5.8 to 18.5 °C, with an average temperature (Tmed) of 2.7 ± 1.2 °C (Table 2). An amount of 842.5–1521.8 chilling hours was accumulated during the 89–100 days of dormancy. The beginning of budburst (53 BBCH), marked by the appearance above the cataphylls of about a 5 mm green tip (Figure 1), was recorded between 3 March (‘Nero’, 2019) and March 12 (‘Nero’, 2021). As shown in Table 2, starting from January 1 to the bud burst (BBCH 53), 65.8 days were counted, with a mean deviation of 2.8 days (CV = 4.2%) and 693.6 ± 68.6 chill hours accumulated. From January 1 to bud burst (BBCH 53), Tmin recorded an oscillation between −4.10 and −2.62 °C, Tmax rose from 6.6 to 10.5 °C, and Tmed ranged in the interval 0.8–2.9 °C (Table 2). The average number of days from 1 January to the phenophases BBCH61, BBCH 71 and BBCH 87 was, respectively, 111.89 ± 6.5 days (CV = 5.8%), 123.5 ± 6.2 days (CV = 5.0%), and 220.7 ± 7.9 days (CV = 3.6%). From the bud burst stage (BBCH 53) to the fruit ripening ending (BBCH 87), 153.8 ± 6.1 days elapsed; the earliest phenophase fruit ripening occurred on July 28 (‘Nero’, 2020), while the latest has occurred on August 20 (‘Melrom’, 2021).
Over the period from bud burst (BBCH 53) till the fruit ripening end (BBCH 87), the average air temperature oscillated around 16.1 °C with a standard deviation of 1.1 °C, the thermal extremes varied between −6.2 °C and 36.8 °C, and heat accumulation was 1702.37 ± 104.91 °C. The average total solar radiation was 245.1 ± 3.8 W/m2. Starting from bud burst (BBCH 53), the beginning of flowering (BBCH 61) started after the accumulation of 181.1 ± 63.7 °C heat and, up to the size of the fruit up to 3 mm (BBCH 71), the heat accumulation was 296.9 ± 14.4 °C (Table 2).
Regarding the influence of late frosts on spring phenophases, in the present study, the bud burst (BBCH 53) occurred in the first half of March, and the full flowering (BBCH 65) began after April 18. Late frosts in March and April (absolute minimum temperatures of −6.1 and −6.2 °C in March 2020 and 2021 and −3.9 °C in April 2020, respectively, data not shown), which affected some species fruit buds in orchards, did not damage the two chokeberry cultivars, which went through their budburst at that time.
Over the three years of observations, after the flowering onset, the minimum temperature did not fall below the freezing point. However, according to Butac and Chitu [8], in the Arges region, climatic accidents can be registered between 11–20 April (with a 4% probability), but also between 21–25 April (with a 6.25% probability).
Results regarding the resistance of the chokeberry to low temperatures, to which the late flowering is added, at a time when the danger of spring climates has passed, have been previously reported by Strik et al. [37]. Although it lasts only 10–12 days, the chokeberry flowering is staggered. By adopting such a strategy, the plants increase their chances of successful pollination in spring, and under conditions of low temperatures (which can affect the evolution of the pollen tube), rain, and wind (which prevents pollination, especially the entomophilic one). This species is self-fertile, which is an advantage given the existence of a small number of cultivars. A similar, staggered flowering strategy has been described by Quesada et al. [38] for a species of Bombacaceae that opens a small number of flowers every day. The staggered flowering of the chokeberry ensured the success of pollination, especially in 2021, when the maximum temperature rose to 28.4 °C (Table 1). In fact, over the three years of study, the absolute maximum temperature recorded during flowering exceeded 25.0 °C (data are not shown). This should be carefully considered because, according to Chitu et al. [19], temperatures exceeding 24–25 °C during flowering are very harmful, causing the stigma to dry out and thus preventing pollen germination.
It was also observed that the timing of phenological stages in the chokeberry species showed significant correlations with climatic variables, such as air temperature and total solar radiation (Table 3). Beaubine et al. [39], too, believe that the timing of spring flowering and leafing of perennials is largely controlled by accumulating temperature.
According to the data presented in Table 3, prolonged vernalization and bud swelling were correlated with the increase in Tmin and Tmed between November 1 and bud burst (BBCH 53; rTmin = 0.775, p = 0.000, rTmed = 0.620, p = 0.006). The analysis of phenophases onset moments, starting from January 1, revealed the highest correlation with Tmin (0.900–0.992, p = 0.000). Thus, a delay in the onset of phenophases correlated with the increase in Tmin was registered. In this context, the delay in the beginning of flowering (BBCH 61), a fruit size up to 3 mm (BBCH 71) and fruit ripe for picking (BBCH 87) appears to be a consequence of the delay in previous phenophases. The bud burst and fruit ripe for picking (BBCH 53–87) phenological range extended in correlation with the increase of Tmin (rTmin = 0.926, p = 0.000), and it was negatively correlated with TSR (r = −0.472, p = 0.048). Positive significant correlations were found between 61 and 53 BBCH (r = 0.906 ***), 71 and 53 BBCH (r = 0.842 ***), 71 and 61 BBCH (r = 0.973 ***), 87 and 53 BBCH (r = 0.509 *), 87 and 61 BBCH (r = 0.695 ***), 87 and 71 BBCH (r = 0.728 ***), respectively (Table 4), and indicated that the late onset of phenophases was preceded by the delayed onset of previous phenophases. Neither the flowering (BBCH 61–71), nor the development and maturation of the fruit (BBCH 71–87), were correlated with the duration length or the onset time of previous phenophases, except for the dormancy and bud burst period (November 1—BBCH 53). In this case, shorter flowering, fruit development and maturation phases followed the prolonged 1 November—bud burst (BBCH 53) interval (r = −0.563 *, −0.517 *, Table 4).
The study of the correlations between the phenophase timing and the previous oscillations in climatic parameters (Table 5) indicated that the higher temperatures during the dormancy and swelling were correlated with the longer bud burst—beginning of flowering period (BBCH 53–61; rTmax = 0.003, p = 0.992) and with the shorter period of beginning of flowering—fruit size up to 3 mm (BBCH 61–71; rTmax = −0.488, p = 0.040) and fruit size up to 3 mm—fruit ripe for picking period (BBCH71–87; rTmax = −0.827, p = 0.000). However, a shorter period of beginning of flowering—fruit size up to 3 mm (BBCH 61–71) was observed after the increase in TSR during bud burst—beginning of flowering (BBCH 53–61), while the Tmin increasing during flowering led to a shorter maturation time (Table 5). In the Arges area, the ripe fruits can be harvested over a 6-week interval. After that, the fruit became visibly dehydrated, but without abscission. Thus, harvesting can be planned based on the dynamics of the level of biologically active components, and also the degree of the dehydration of chokeberry fruits [3].
4. Conclusions
The present study indicated that chokeberry phenology is a dynamic process, which developed in correlation with the ambient temperature and total solar radiation. The chokeberry-flowering strategy and the restricted correlations of flowering duration with temperature and TSR may be the result of the species’ adaptation, gained over time. During dormancy, the decreasing in minimum temperature to −14.1 °C, just like the temperatures of −6.2 °C during bud burst, did not cause any damage to the chokeberry crop. In addition, resistance to high summer temperatures gave the chokeberry the characteristics of a species with a high potential for adaptation to a constantly changing climate. The flowering timing was shortened as a result of the increase in maximum temperature and total solar radiation. The development of phenophases indicates that A. melanocarpa is a species adapted to the temperate continental climate of southern Romania. Further studies will be carried out in order to follow up on the phenological changes under the current climate change and also to formulate additional recommendations for the sustainable management of this crop.
Author Contributions
Conceptualization, S.C.; investigation, M.D.D. and I.E.M.; writing—original draft, S.C., M.D.D. and I.E.M.; writing—review and editing, S.C. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Skvortsov, A.K.; Maitulina, Y.K. On distinctions of cultivated black-fruited aronia from its wild ancestors. Bull. Cent. Bot. Garden 1982, 126, 35–40. [Google Scholar]
- Brand, M.H. Breeding better aronia plants©. Acta Hortic. 2014, 1055, 269–272. [Google Scholar] [CrossRef] [Scilit]
- Mazilu, I.E.; Paraschiv, M.; Dinu, M.D.; Cosmulescu, S.N. Biochemical changes in two Aronia melanocarpa cultivars’ berries during the harvest season. Not. Bot. Horti. Agrobo. 2021, 49, 12393. [Google Scholar] [CrossRef] [Scilit]
- Bussieres, J.; Boudreau, S.; Clément–Mathieu, G.; Dansereau, B.; Rochefort, L. Growing black chokeberry (Aronia melanocarpa) in cut-over peatlands. HortScience 2008, 43, 494–499. [Google Scholar] [CrossRef] [Scilit]
- Vinogradova, Y.; Pergl, J.; Essl, F.; Hejda, M.; van Kleunen, M.; Pyšek, P. Invasive alien plants of Russia: Insights from regional inventories. Biol. Invasions 2018, 20, 1931–1943. [Google Scholar] [CrossRef] [Scilit]
- Leostrin, A.; Pergl, J. Alien flora in a boreal region of European Russia: An example of Kostroma oblast. Biol. Invasions 2021, 23, 3337–3350. [Google Scholar] [CrossRef] [Scilit]
- Rosca, I.; Donea, V.; Donea, E.; Dadu, C.; Sava, P. Aronia melanocarpa (Michx.) Elliot. cultură de perspectivă pentru Republica Moldova. Pomic. Vitic. Vinif. 2019, 81, 50–57. [Google Scholar]
- Butac, M.; Chitu, E. Impactul schimbărilor climatice asupra dinamicii fenologice a unor soiuri de prun cultivate în bazinul pomicol Argeș. Fruit Grow. Res. 2007, XXIII. Available online: https://publications.icdp.ro/ (accessed on 15 February 2022).
- Cosmulescu, S.; Baciu, A.; Botu, M.; Achim, G. Environmental factors’ influence on walnut flowering. Acta Hortic. 2010, 861, 83–88. [Google Scholar] [CrossRef] [Scilit]
- Cosmulescu, S.; Calusaru, F.G. Influence of temperature on blackthorn (Prunus spinosa L.) phenophases in spring season. J. Agric. Meteorol. 2020, 76, 53–57. [Google Scholar] [CrossRef] [Scilit]
- Cosmulescu, S.; Ștefănescu, D.; Stoenescu, A.M. Variability of phenological behaviours of wild fruit tree species based on discriminant analysis. Plants 2022, 11, 45. [Google Scholar] [CrossRef] [Scilit]
- Birsanu Ionescu, M.; Cosmulescu, S.N. Effect of climatic conditions on flowering of walnut genotypes in Romania. J. Nuts 2017, 8, 161–167. [Google Scholar]
- Cosmulescu, S.; Ionescu, M.B. Phenological calendar in some walnut genotypes grown in Romania and its correlations with air temperature. Int. J. Biometeorol. 2018, 62, 2007–2013. [Google Scholar] [CrossRef] [Scilit]
- Khodorova, N.V.; Boitel-Conti, M. The role of temperature in the growth and flowering of geophytes. Plants 2013, 2, 699–711. [Google Scholar] [CrossRef] [Scilit]
- Penso, G.A.; Citadin, I.; Scariotto, S.; Santos, C.E.; Junior, A.W.; Bruckner, C.H.; Rodrigo, J. Development of peach flower buds under low winter chilling conditions. Agronomy 2020, 10, 428. [Google Scholar] [CrossRef] [Scilit]
- Paltineanu, C.; Chitu, E. Climate change impact on phenological stages of sweet and sour cherry trees in a continental climate environment. Sci. Hortic. 2020, 261, 109011. [Google Scholar] [CrossRef] [Scilit]
- Durant, J.M.; Hjermann, D.Ø.; Anker-Nilssen, T.; Beaugrand, G.; Mysterud, A.; Pettorelli, N.; Stenseth, N.C. Timing and abundance as key mechanisms affecting trophic interactions in variable environments. Ecol. Lett. 2005, 8, 952–958. [Google Scholar] [CrossRef] [Scilit]
- Chuine, I. Why does phenology drive species distribution? Phil. Trans. R. Soc. 2010, 365, 3149–3160. [Google Scholar] [CrossRef] [Scilit]
- Chitu, E.; Butac, M.; Chitu, V. Modelling of climatic changes impact on the growth and fruiting of some plum cultivars in the southern part of Romania. Acta Hortic. 2012, 968, 253–260. [Google Scholar] [CrossRef] [Scilit]
- Stucky, B.J.; Guralnick, R.; Deck, J.; Denny, E.G.; Bolmgren, K.; Walls, R. The plant phenology ontology: A new informatics resource for large-scale integration of plant phenology data. Front. Plant Sci. 2018, 9, 517. [Google Scholar] [CrossRef] [Scilit]
- Ulrich, J.; Bucher, S.F.; Eisenhauer, N.; Schmidt, A.; Türke, M.; Gebler, A.; Römermann, C. Invertebrate decline leads to shifts in plant species abundance and phenology. Front. Plant Sci. 2020, 11, 1410. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tresson, P.; Brun, L.; Cortazar-Atauri, I.G.; Audergon, J.M.; Buléon, S.; Chenevotot, H.; Launay, M. Future development of apricot blossom blight under climate change in Southern France. Eur. J. Agron. 2020, 112, 125960. [Google Scholar] [CrossRef] [Scilit]
- Ekholm, A.; Tack, A.J.; Pulkkinen, P.; Roslin, T. Host plant phenology, insect outbreaks and herbivore communities–The importance of timing. J. Anim. Ecol. 2020, 89, 829–841. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chitu, E.; Paltineanu, C. Timing of phenological stages for apple and pear trees under climate change in a temperate-continental climate. Int. J. Biometeorol. 2020, 64, 1263–1271. [Google Scholar] [CrossRef] [Scilit]
- Nicola, C.; Florea, A.; Chițu, E.; Butac, M. Evaluation of the biochemical quality of Aronia melanocarpa fruits in the conditions of southern Romania, under the influence of fertilization. Sci. Pap. Ser. B Hortic. 2020, 64, 147–154. [Google Scholar]
- Meier, U. Growth Stages of Mono- and Dicotyledoneus Plants. BBCH Monograph, 2nd ed.; Federal Biological Research Centre for Agriculture and Forestry: Braunschweig, Germany, 2001; Available online: https://www.julius-kuehn.de/media/Veroeffentlichungen/bbch%20epaper%20en/page.pdf (accessed on 18 February 2022).
- Coman, M.; Chițu, E. Zonarea Speciilor Pomicole În Funcție De Condițiile Pedoclimatice Şi Socioeconomice Ale României. Editura Invel Mutimedia, Piteşti. 2014. Available online: https://icdp.ro/wp-content/uploads/2020/09/Zonarea-speciilor-pomicole.pdf (accessed on 15 February 2022).
- Weinberger, J.H. Chilling requirements of peach varieties. J. Am. Soc. Hortic. Sci. 1950, 56, 122–128. [Google Scholar]
- Luedeling, E.; Kunz, A.; Blanke, M.M. Identification of chilling and heat requirements of cherry trees a statistical approach. Int. J. Biometeorol. 2013, 57, 679–689. [Google Scholar] [CrossRef] [Scilit]
- Ruiz, D.; Campoy, J.A.; Egea, J. Chilling and heat requirements of apricot cultivars for flowering. Environ. Exp. Bot. 2007, 61, 254–263. [Google Scholar] [CrossRef] [Scilit]
- Črepinšek, Z.; Štampar, F.; Kajfež-Bogataj, L.; Solar, A. The response of Corylus avellana L. phenology to rising temperature in north-eastern Slovenia. Int. J. Biometeorol. 2012, 56, 681–694. [Google Scholar] [CrossRef] [Scilit]
- González-Ubierna, S.; Lai, R. Modelling the effects of climate factors on soil respiration across Mediterranean ecosystems. J. Arid Environ. 2019, 165, 46–54. [Google Scholar] [CrossRef] [Scilit]
- Morin, X.; Augspurger, C.; Chuine, I. Process-based modeling of species’distributions: What limits temperate tree species’range boundaries? Ecology 2007, 88, 2280–2291. [Google Scholar] [CrossRef] [Scilit]
- Moore, L.M.; Lauenroth, W.K. Differential effects of temperature and precipitation on early-vs. late-flowering species. Ecosphere 2017, 8, e01819. [Google Scholar] [CrossRef] [Scilit]
- Cho, L.H.; Yoon, J.; An, G. The control of flowering time by environmental factors. Plant J. 2017, 90, 708–719. [Google Scholar] [CrossRef] [Scilit]
- Kazan, K.; Lyons, R. The link between flowering time and stress tolerance. J. Exp. Bot. 2016, 67, 47–60. [Google Scholar] [CrossRef] [Scilit]
- Strik, B.; Finn, C.; Wrolstad, R. Performance of chokeberry (Aronia melanocarpa) in Oregon, USA. Acta Hortic. 2003, 626, 439–443. [Google Scholar] [CrossRef] [Scilit]
- Quesada, M.; Fuchs, E.J.; Lobo, J.A. Pollen load size, reproductive success, and progeny kinship of naturally pollinated flowers of the tropical dry forest tree Pachira quinata (Bombacaceae). Am. J. Bot. 2001, 88, 2113–2118. [Google Scholar] [CrossRef] [Scilit]
- Beaubien, E.G.; Hall-Beyer, M. Plant phenology in western Canada: Trends and links to the view from space. Environ. Monit. Assess. 2003, 88, 419–429. [Google Scholar] [CrossRef] [Scilit]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).