Article

Geodiversity and Ecological Filtering Drive High Local Diversity of Inga (Fabaceae) in Imbabura, Northern Ecuadorian Andes


by
Hugo Orlando Paredes Rodríguez
1,
Wilfredo Ramiro Franco
2,* and
Elio Sanoja
3
1
Facultad de Ingeniería en Ciencias Agropecuarias y Ambientales, Universidad Técnica del Norte, Ibarra 100105, Ecuador
2
Facultad de Ciencias de la Tierra y Agua, Universidad Regional Amazónica Ikiam, Tena 150150, Ecuador
3
Postgrado en Ciencias Ambientales, Universidad Nacional Experimental de Guayana, Puerto Ordaz, Ciudad Guayana 8051, Venezuela
*
Author to whom correspondence should be addressed.
Forests 2026, 17(4), 508; https://doi.org/10.3390/f17040508
Submission received: 27 February 2026 / Revised: 19 March 2026 / Accepted: 24 March 2026 / Published: 20 April 2026
(This article belongs to the Section Forest Biodiversity)

Abstract

The neotropical genus Inga (Fabaceae) is a fast-growing tree component of tropical forests which plays crucial ecological and functional roles. However, its diversity patterns and the specific environmental drivers that structure its distribution in Andean landscapes remain insufficiently documented. This study aimed to quantify the diversity and distribution of Inga species in the province of Imbabura (4785 km2), northern Ecuador, while evaluating the influence of key environmental determinants. By integrating 52 field records along 321 km of exploration and 22 herbarium records (QCNE, MO, AAU, F, HUTN), the study analyzes the role of topographic variables (12.5 m resolution) and climate data (1 km2 resolution). Seventeen species were recorded, almost tripling previous regional findings. The results demonstrate that species richness and occurrence are strongly structured by altitude, temperature, and soil properties as primary environmental drivers. Ten species showed narrow altitudinal ranges and limited thermal tolerance (<2 °C), indicating high habitat specialization, while I. densiflora and I. insignis exhibited broader niches. Edaphically, most species were associated with sandy loam soils, particularly Mollisols and Inceptisols developed from volcanic material. These findings indicate that climatic gradients and edaphic conditions act as the main environmental filters shaping Inga assemblages in heterogeneous montane landscapes. The observed high level of specialization suggests significant vulnerability to land-use change and highlights the need for habitat-specific conservation strategies in Andean forests.

1. Introduction

Tree diversity is critical to the health of the global ecosystem. South America is home to remarkable richness, with approximately 16,880 tree species, a figure that significantly exceeds the diversity found in North America (1873), Africa (3529), and Oceania (4560) [1]. Within this context, Ecuador stands out as a biodiversity hotspot, harboring approximately 2500 recognized tree species [2]. This high level of species richness is not only a biological hallmark but also the foundation for essential ecosystem services, including carbon sequestration, hydrological regulation, and the maintenance of complex biotic interactions that sustain Andean forest stability.
Despite its ecological importance, this biodiversity faces critical and escalating threats. Ecuador, in particular, confronts a severe environmental challenge: persistent deforestation. Between 1990 and 2000, the average deforestation rate was approximately 89,944 ha·year−1 (−0.71%), and although this rate decreased to 44,497 ha·year−1 (−0.37%) between 2008 and 2014, the continued loss of forest cover and subsequent habitat degradation represent major challenges for biodiversity conservation and ecosystem sustainability [3]. This trend is particularly evident in the province of Imbabura, where 2.8 kha (2.0% of the total forest cover) were deforested between 2002–2024 [4]. These anthropogenic pressures, translated into land-use changes, drive habitat fragmentation, isolating populations and threatening the survival of specialized taxa.
In this context, the genus Inga Mill. (Fabaceae) is particularly relevant. It is a diverse group of legumes common in neotropical forests with important socioeconomic value [5]. The genus includes around 300 species distributed from Mexico to northern Argentina, with the highest diversity in the Andes of Peru, Ecuador and Colombia [5]. In Ecuador, publications such as “Trees of Ecuador” describe representative species [6], while the fundamental work of Pennington and Revelo reports 75 species for the country. However, historically only six species have been reported for the province of Imbabura [7], a figure that contrasts with the heterogeneous relief and the potential for numerous ecological niches of the region.
The presence and development of Inga species are conditioned by complex environmental drivers, where altitude, precipitation, and temperature act as primary physiological filters, while soil properties determine edaphic specialization [8]. However, human occupation in South America has driven the domestication of plants for millennia, modifying landscapes since pre-Columbian times [9,10]. Moreover, the consumption of Inga fruits (guabas) influence dispersion, with humans acting as vectors along roads and trails. This phenomenon contrasts with the behavior of wild species, which tend to remain confined to forest remains [7]. This duality suggests that the distribution of Inga in Imbabura is driven by a complex interaction between natural environmental drivers and anthropogenic history, where climatic and edaphic variables establish the fundamental niche of the species.
Therefore, it is necessary to deepen the knowledge of the distribution and ecology of Inga species in this Andean region to improve their conservation and sustainable use. The objective of this study is to characterize the diversity and geographic distribution of Inga species in the province of Imbabura, Ecuador, by identifying the key environmental drivers—specifically climatic gradients and edaphic conditions—that shape their occurrence across different Andean ecosystems.
To achieve this objective, this study addresses the following research questions:
RQ1. 
How is the taxonomic richness of the genus Inga distributed across the heterogeneous landscapes of Imbabura?
RQ2. 
Which environmental drivers—climatic or edaphic—exert the greatest influence as ecological filters on species distribution?
RQ3. 
To what extent do Inga species exhibit niche specialization versus ecological plasticity along the Andean altitudinal gradient?

2. Materials and Methods

2.1. Study Area

The study was carried out in the province of Imbabura, located in the northern inter-Andean region of Ecuador, covering the western foothills of the Royal and Western mountain ranges. The region is characterized by a heterogeneous relief composed of slopes, hills and plateaus, shaped by drainage networks and tectonic processes. This geomorphological complexity creates a mosaic of environmental conditions that favor high plant diversity and provides differentiated ecological niches for the Inga genus.

2.2. Data Collection and Sampling Strategy

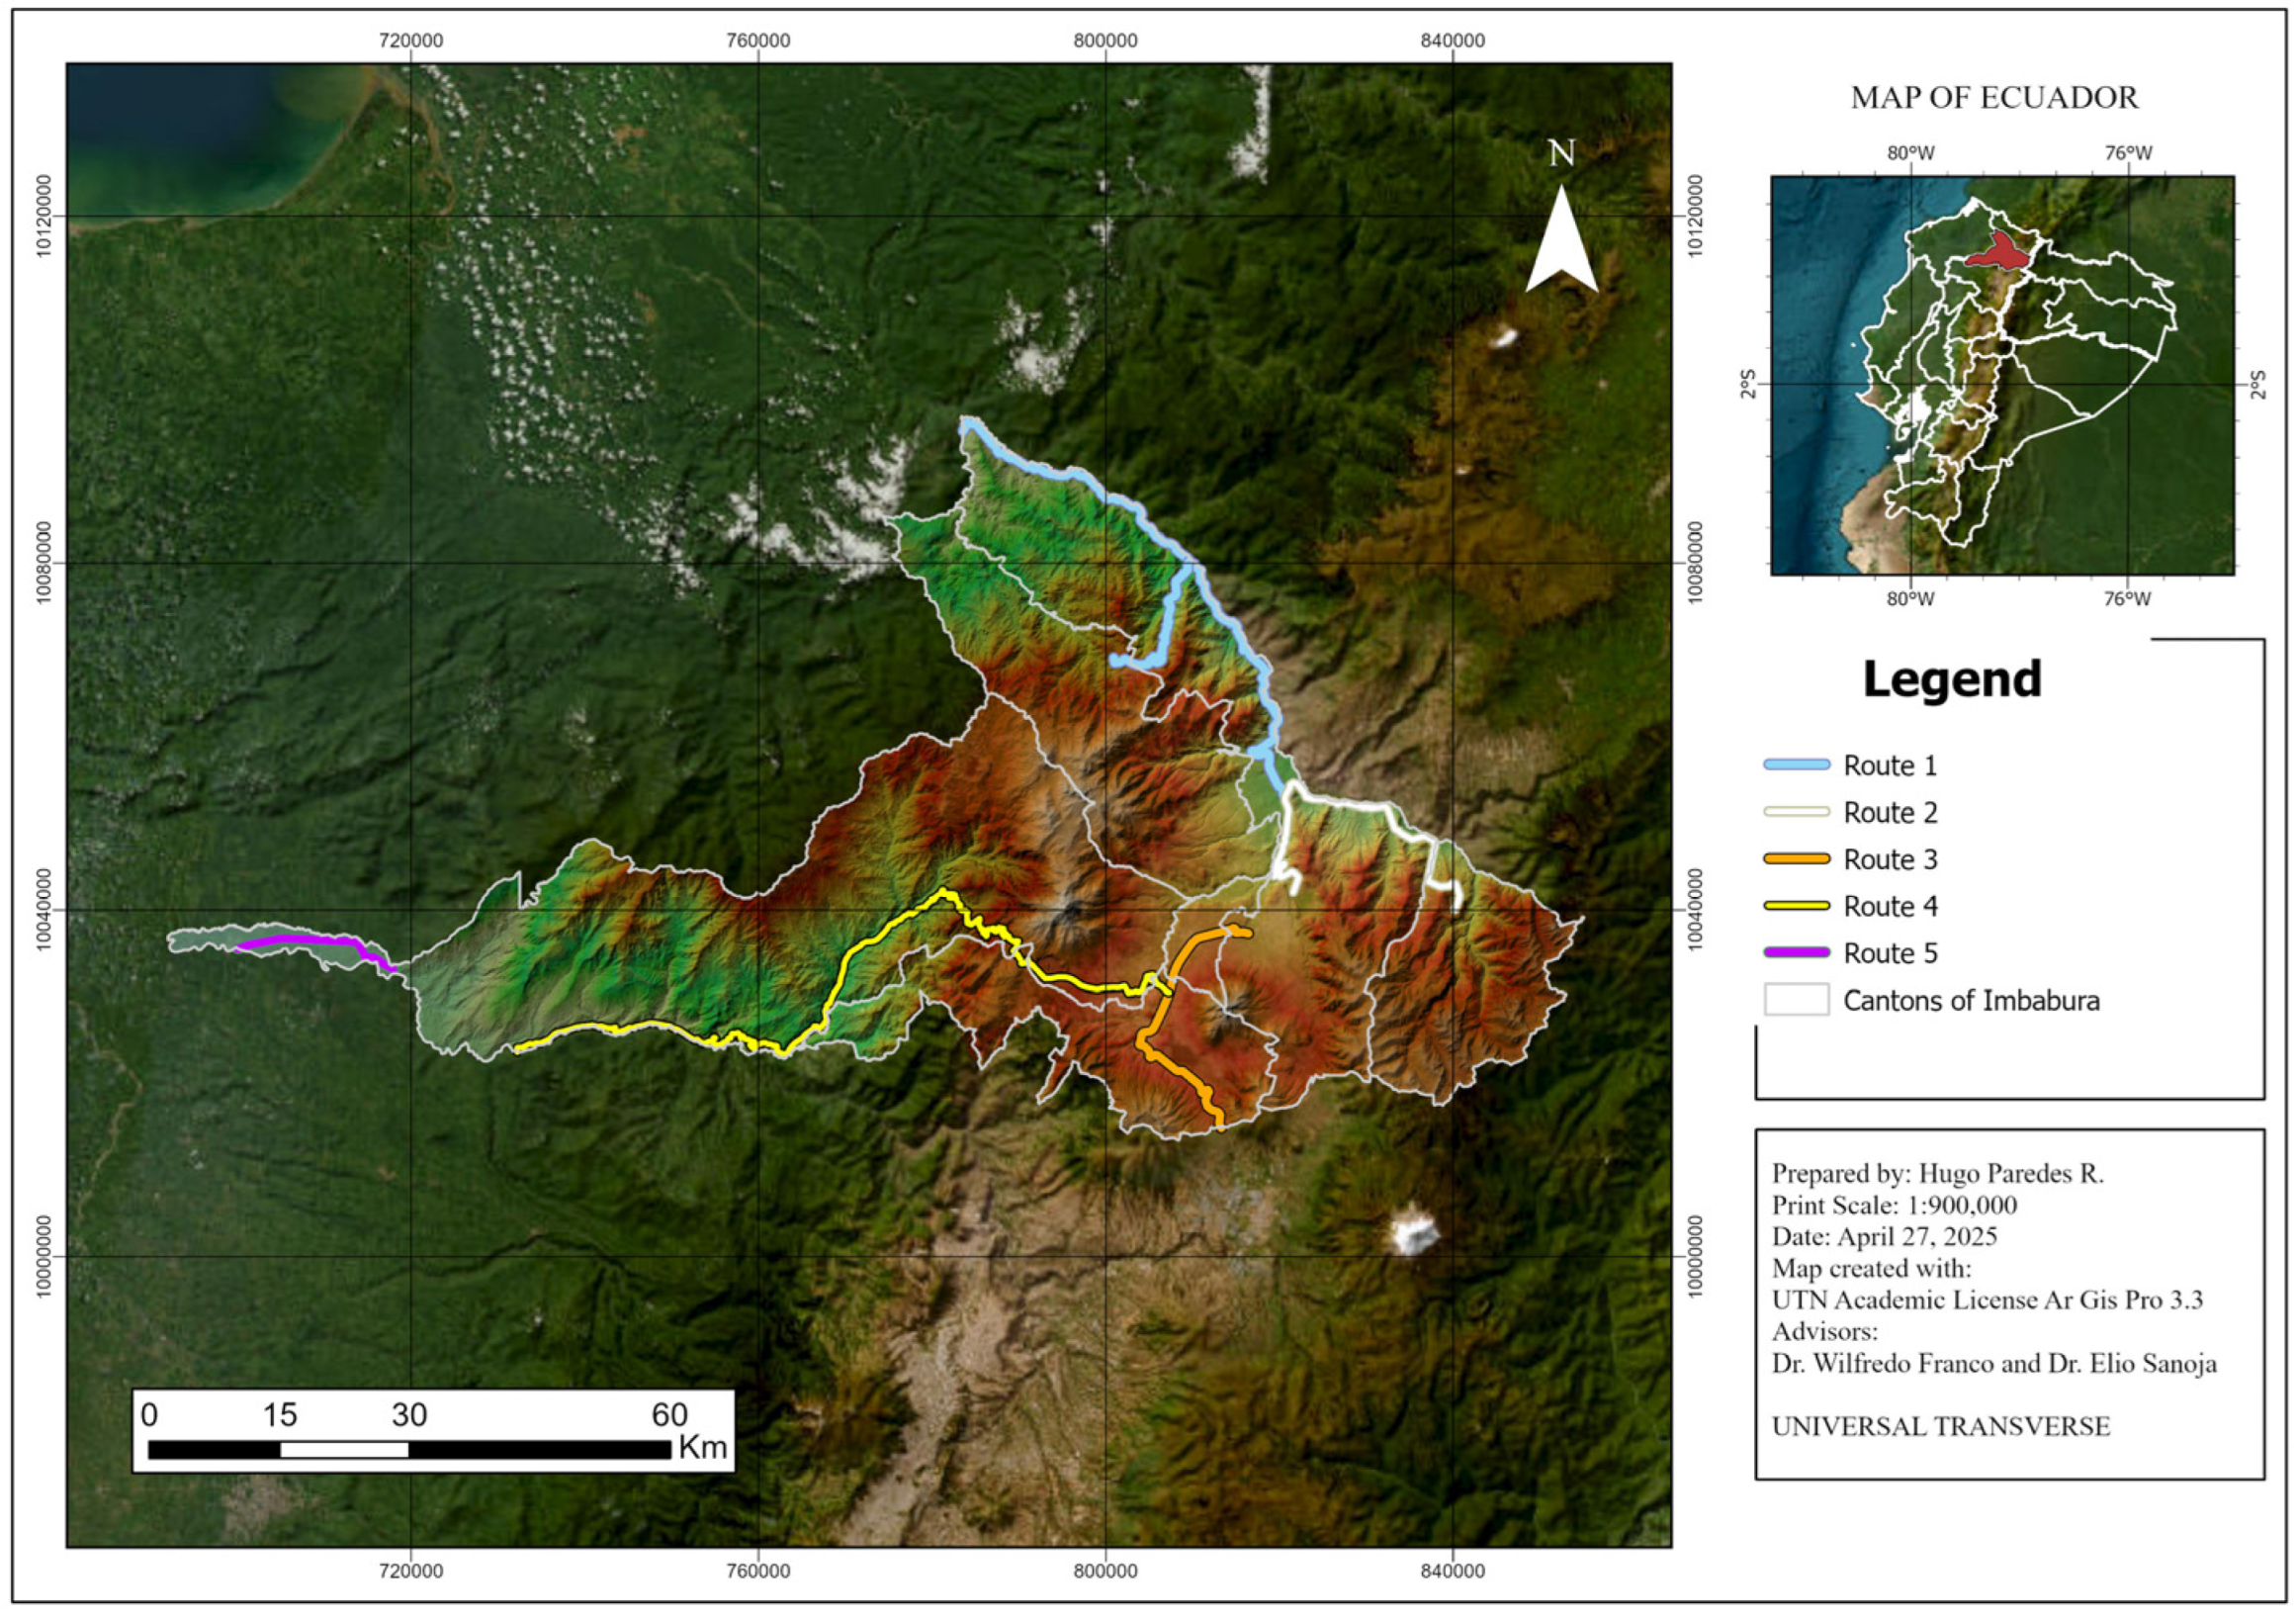
The research methodology followed a stratified opportunistic sampling design. Five exploration routes totaled 321 km, representing the province’s diverse floristic and environmental composition. These routes were chosen based on three main parameters:
Environmental Heterogeneity: Routes were designed to traverse the complete altitudinal gradient of the province, from the subtropical lowlands at 600 m a.s.l. to the high Andean paramo interfaces above 3000 m a.s.l.
Biogeographic Representation: The selection ensured coverage of both the western slopes (influenced by Chocó-Andean humidity) and the drier inter-Andean valleys, capturing the distinct precipitation regimes (500–3500 mm/year) that characterize the region.
Historical and Ecological Relevance: Routes were aligned with areas containing historical records of the genus Inga and those providing access to significant forest remnants where specialized taxa are more likely to persist.
This configuration allowed for a comprehensive assessment of the ecological niches available for the genus across the 4785 km2 of Imbabura (Figure 1).
Sampling was conducted on adult individuals located within a 50 m buffer zone on each side of the road. Collection protocols followed the standards of the Herbarium of the Universidad Técnica del Norte (HUTN). Field data were recorded using the KoBoToolbox application version 2025.3.3 [11], parameterized to capture variables specific to the genus Inga.
In addition to primary data, secondary data from the Global Biodiversity Information Facility (GBIF) (accessed on 28 August 2023 and 20 March 2025) [12,13] and national herbarium databases (QCNE, MO, AAU, F, HUTN) were compiled to identify historical records of Inga in Imbabura. Sites with historical records of species were reviewed for verification. This study was carried out under research permit No. MAATE-ARSFC-2023-0036, granted by the Ministry of Environment, Water and Ecological Transition of Ecuador (MAATE) [14].

2.3. Taxonomic Identification

Botanical samples were processed using traditional phytotaxonomic techniques, which involved the comparative morphological analysis of vegetative and reproductive characters—specifically the arrangement of foliar glands, rachis winging, and fruit morphology. This morphological approach was selected as it constitutes the fundamental standard for the identification of the genus Inga in the Neotropics, where species are largely distinguished by macroscopic structural traits. The taxonomic identification was performed based on (i) specialized dichotomous keys proposed by Pennington & Revelo [7] and Pennington [15]; (ii) Inga specialist validation (Eng. Nixon Revelo); and (iii) comparison with physical specimens at the HUTN herbarium.

2.4. Geospatial and Ecological Analysis

Geospatial analysis was performed using ArcGIS Pro (version 3.3)—https://www.esri.com/es-es/arcgis/products/arcgis-pro/overview (accessed on 23 March 2026). The precise location of each specimen was integrated within the provincial and cantonal administrative limits [16]. To determine the ecological zoning of Inga species, point data was overlaid with geopedological shapefiles containing the following variables:
  • Climatic: temperature, precipitation and an ombrothermal index [17].
  • Edaphic: soil order, texture, pH and slope [18].
  • Land Use: current vegetation cover and types of land use [19].
Data sources included the Ministry of Agriculture and Livestock (MAG) (SIGTIERRAS), the Ministry of the Environment (MAATE) and the National Institute of Meteorology and Hydrology (INAMHI). These variables were analyzed to generate distribution maps and determine the specific ecological niche for each species.
The extraction method (point sampling) includes the extraction of environmental values through exhaustive point sampling or raster data. For the climate, topography, and SoilGrid layers, the “Extract Values to Points” tool was used, assigning the corresponding pixel value to the coordinate of each Inga record. For the SIGTIERRAS and MAATE variables (polygonal data), a spatial intersection (Spatial Join/Overlay) was used, where each record acquired the attributes of the soil or vegetation cover polygon in which it was geographically located. Table 1 presents the environmental variables used in the study.

2.5. Calculation of Thermal Ranges and Environmental Tolerances

  • Identification of the Niche Achieved: Based on species spot sampling, the set of values for Average Annual Temperature (Bio1) and Annual Precipitation (Bio12) corresponding to their coordinates was obtained.
  • Calculation of Thermal Range: The thermal range (ΔT) was defined using the formula ΔT = Tmax − Tmin, where Tmax is the highest and Tmin the lowest temperature recorded for the species.
  • Specialization criterion: Any species whose spatial range was less than 2 °C within the province was classified as a “thermal niche specialist”, indicating that its populations only persist within a very limited thermal range; in contrast, species with (ΔT) > 2 °C were considered “generalists”.

3. Results

3.1. Floristic Composition and Diversity

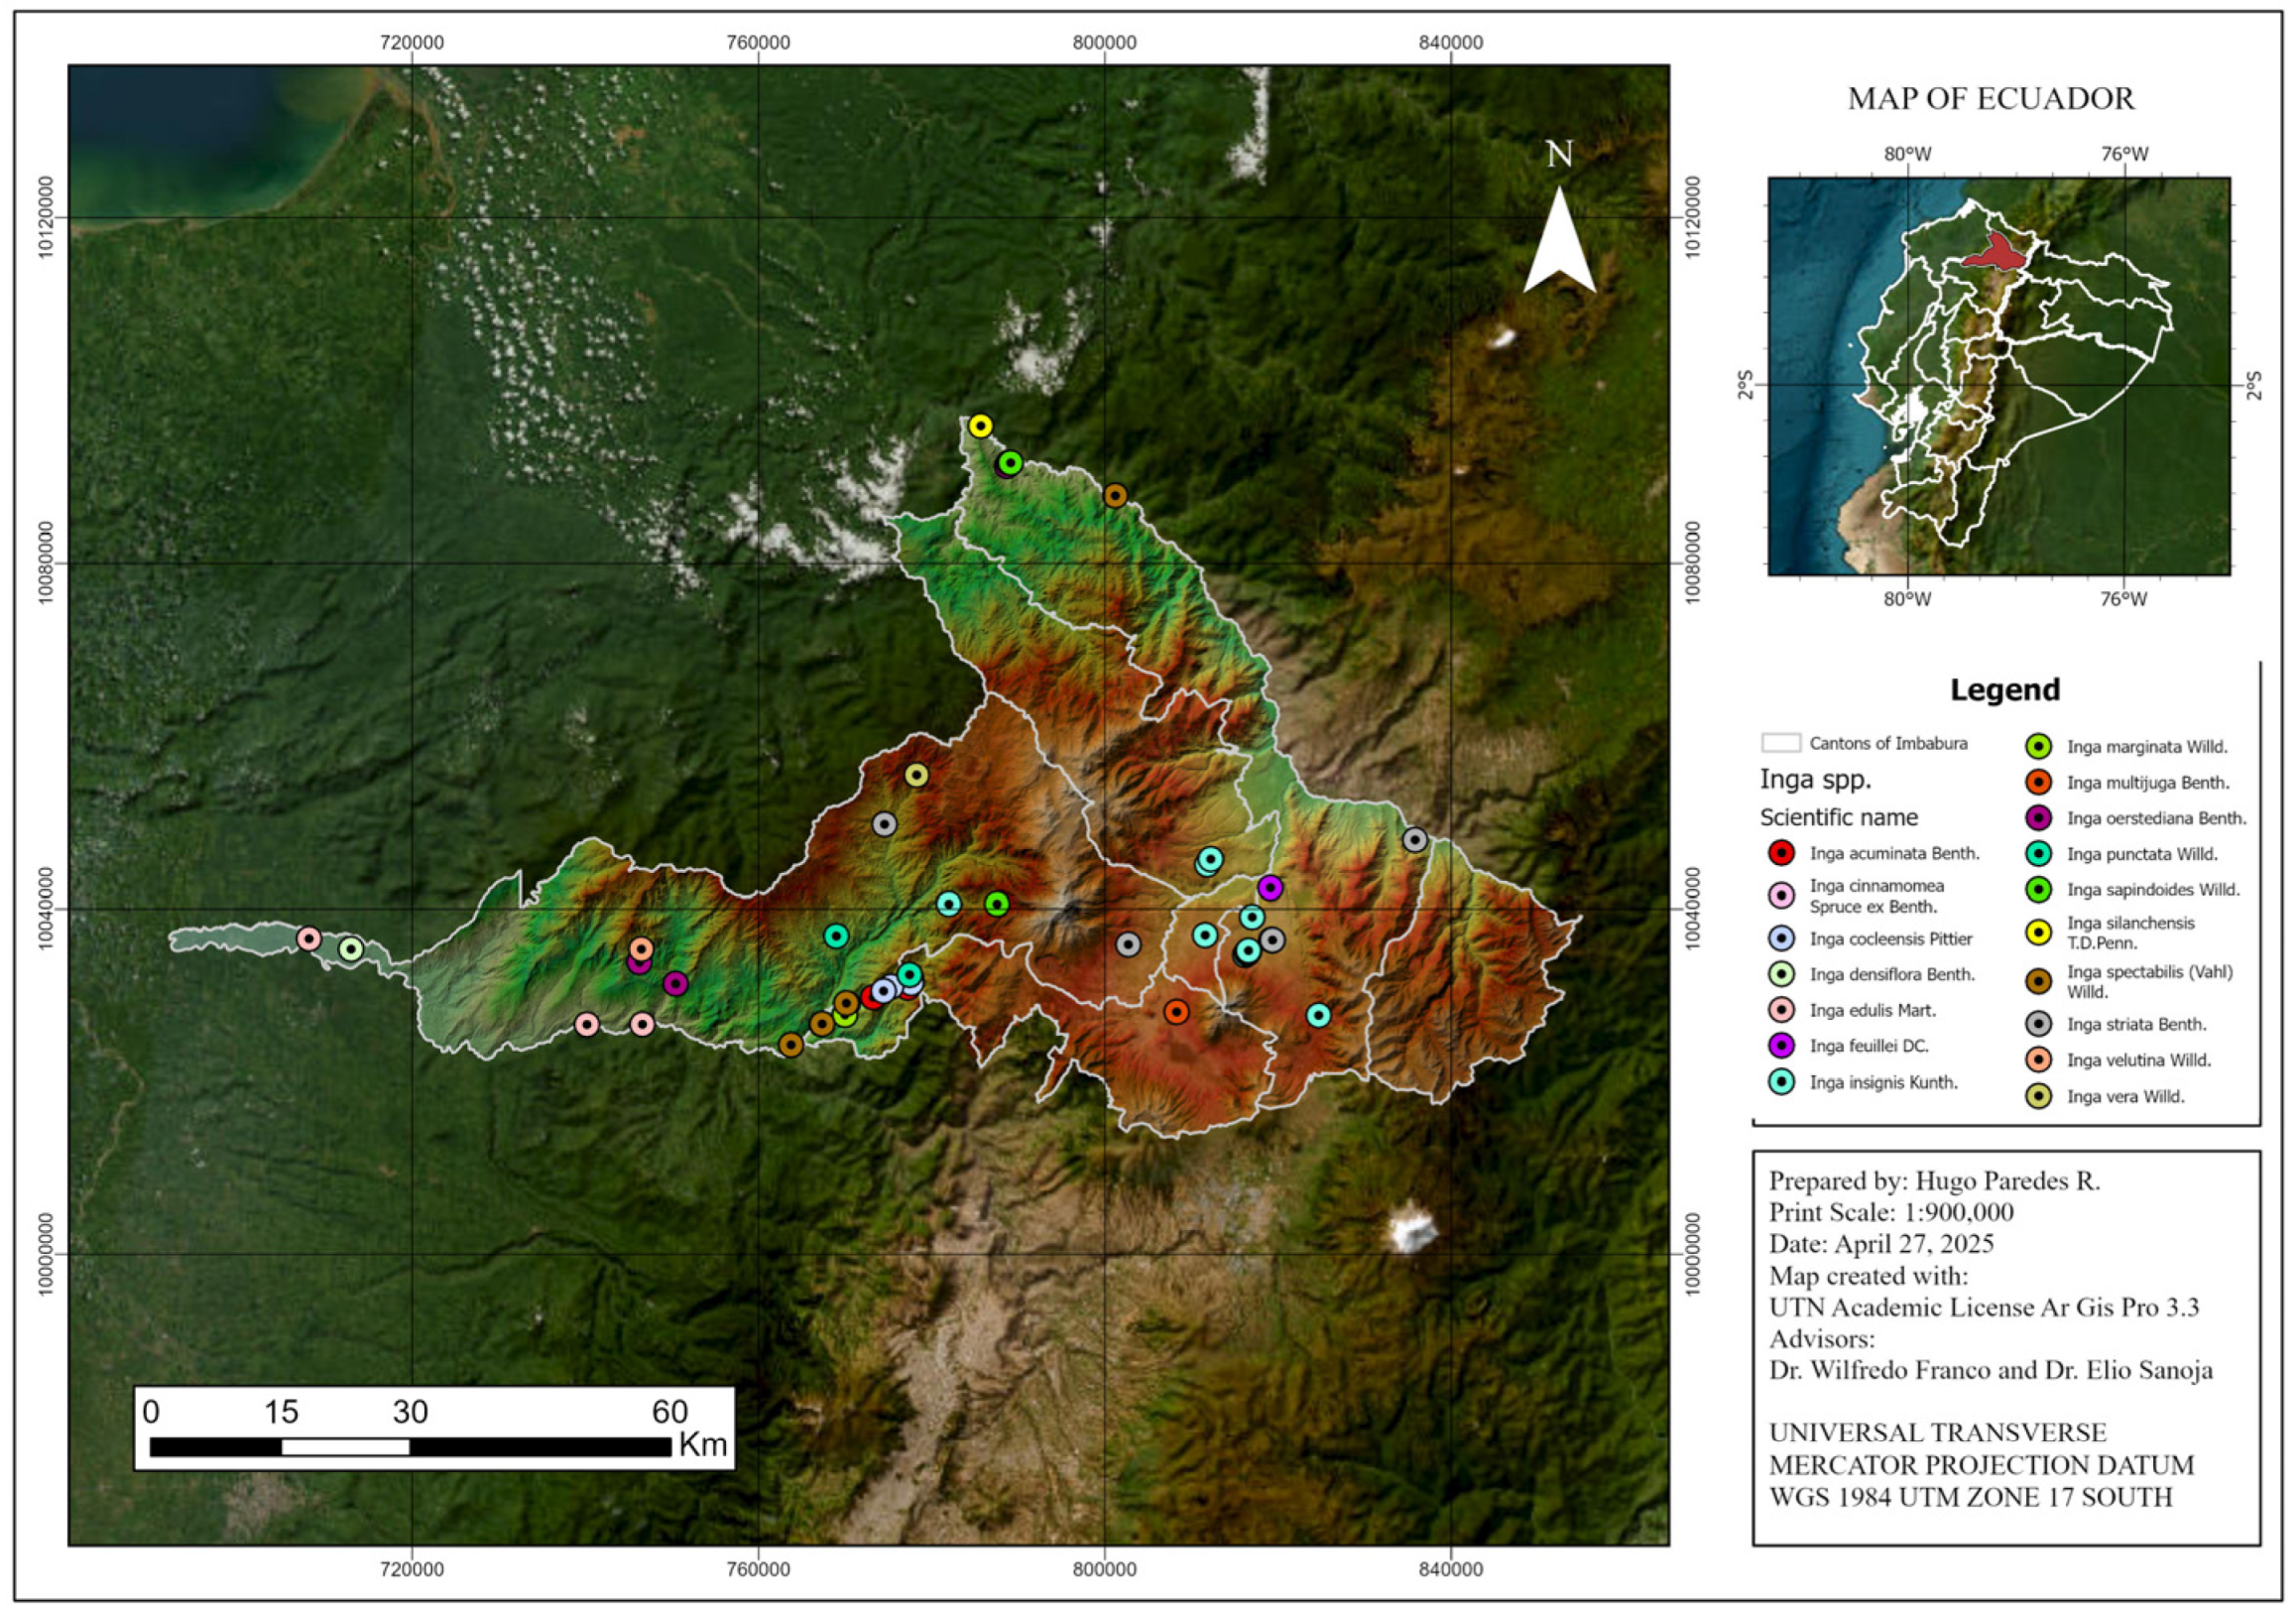
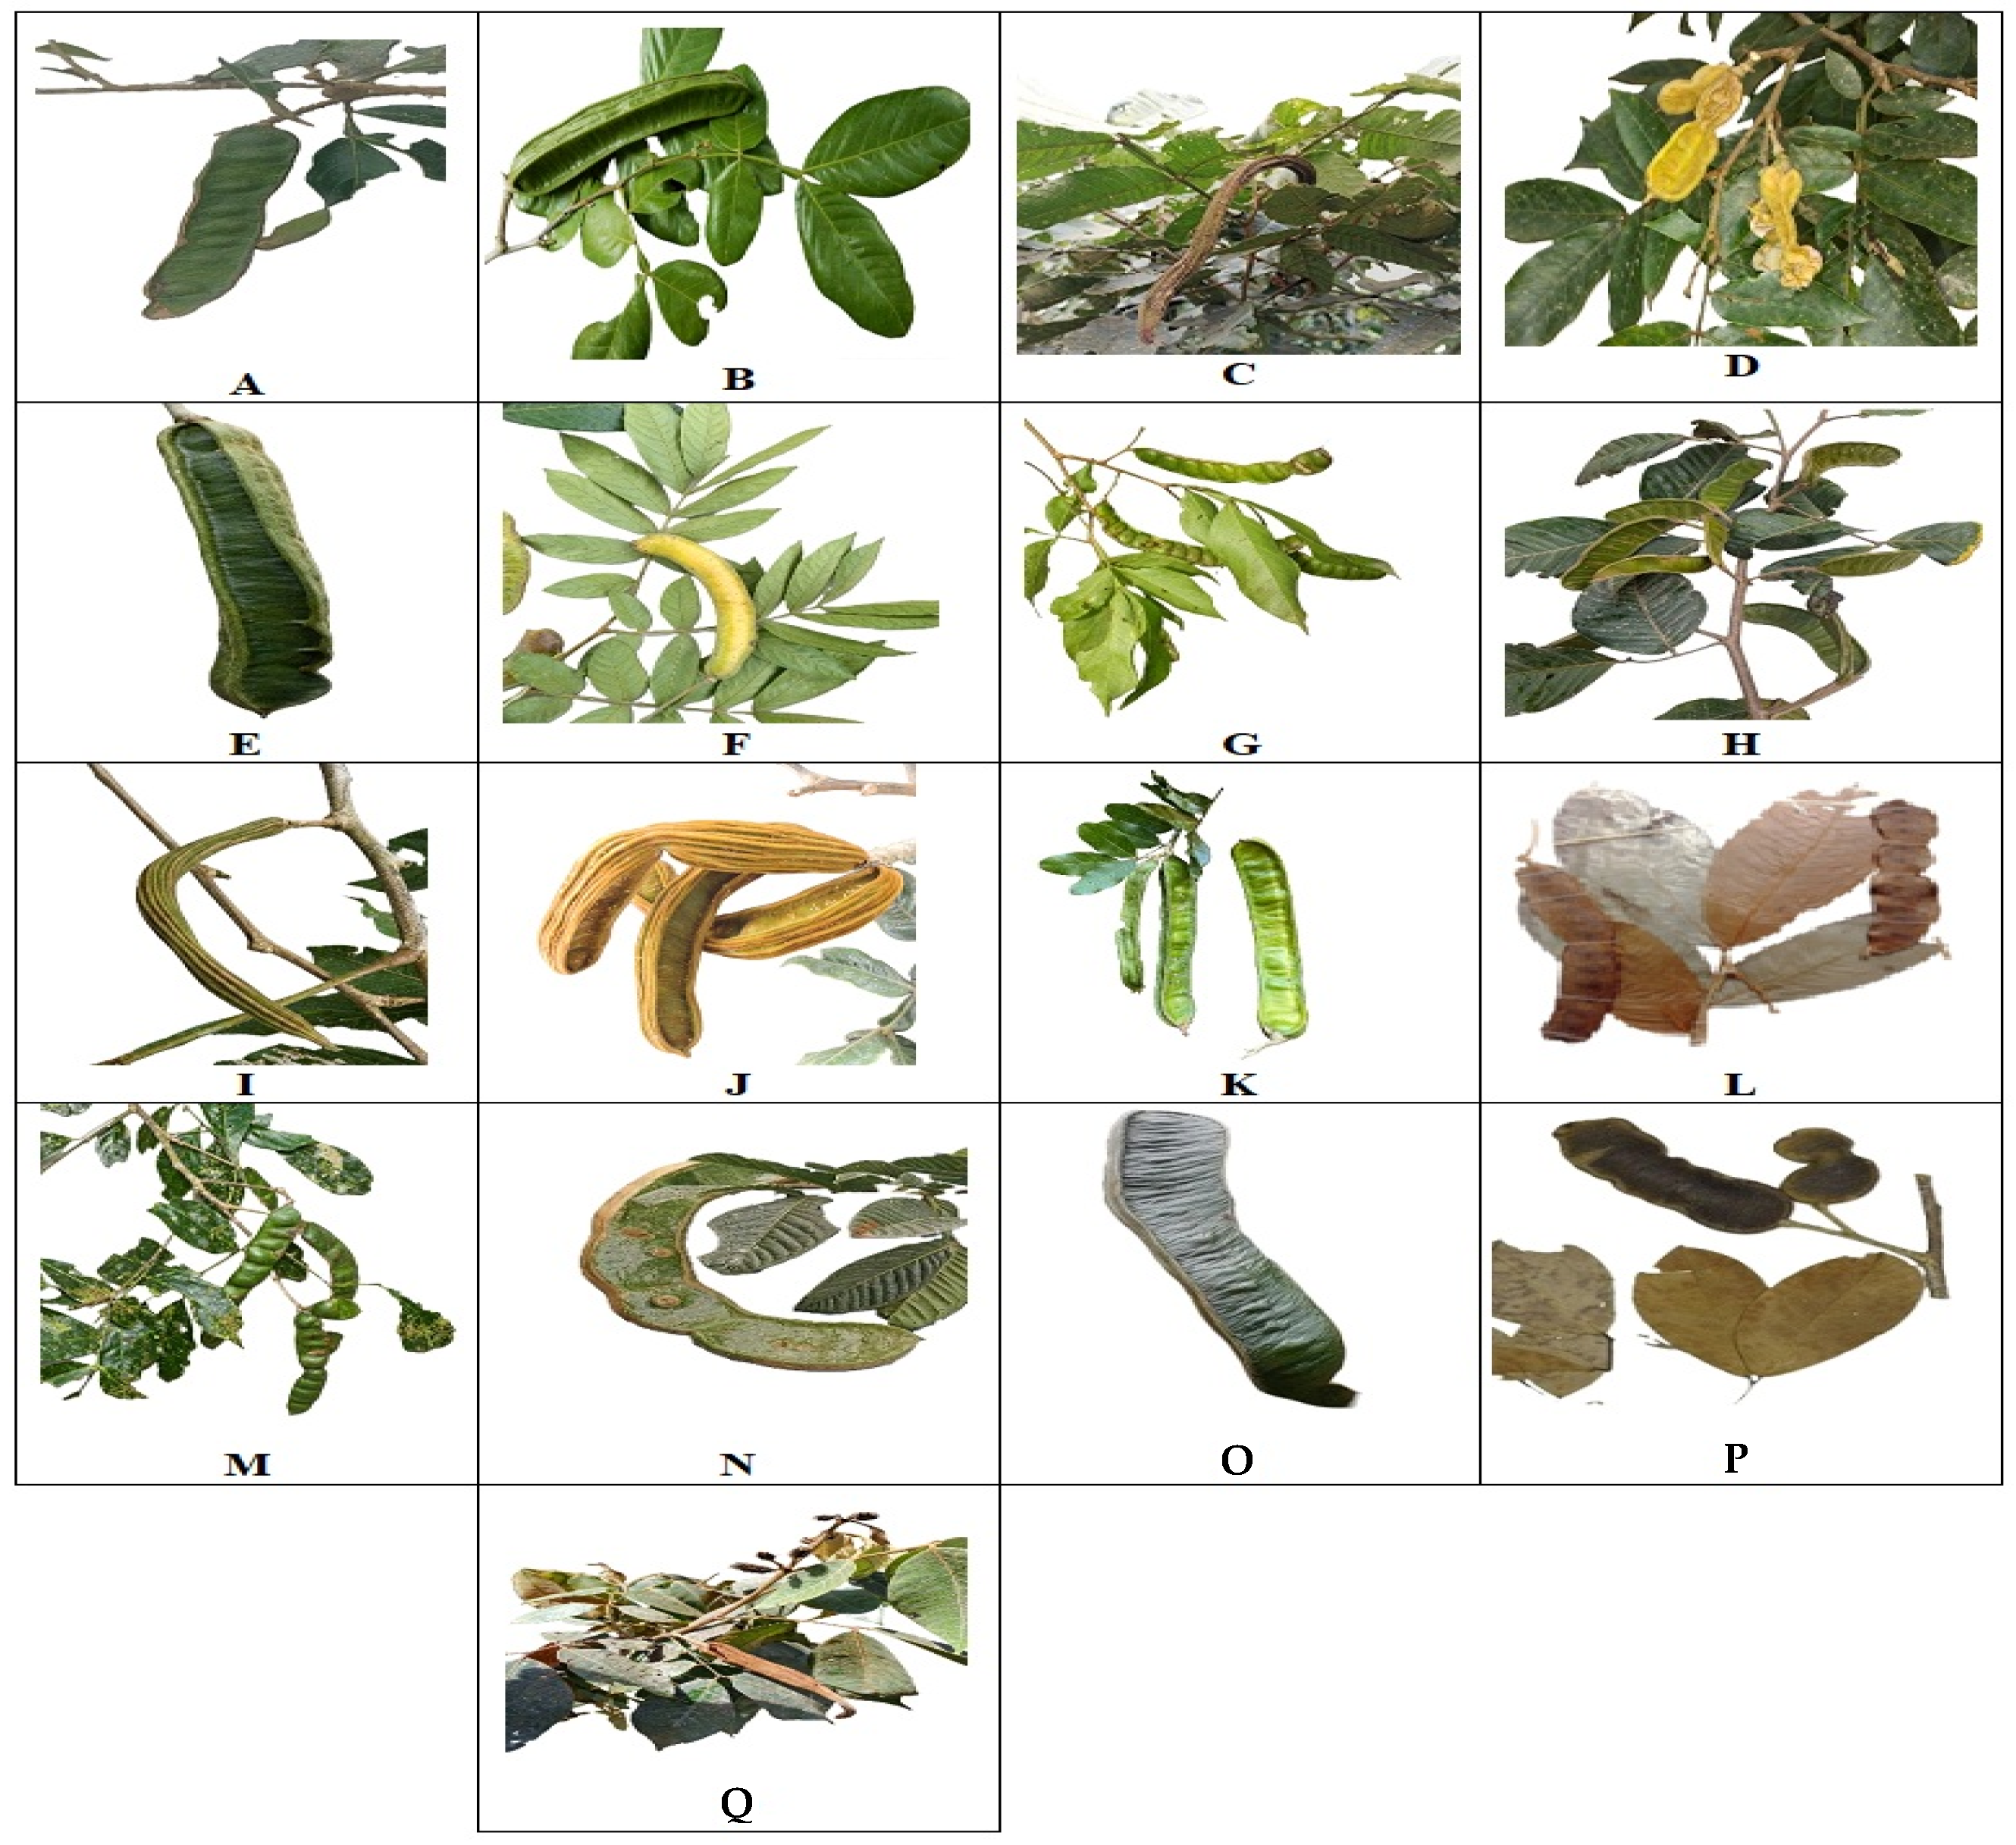
The review of national and international herbaria databases (QCNE, MO, AAU, F, HUTN), combined with systematic field expeditions, confirmed the presence of 17 species of the genus Inga in the province of Imbabura. Of the 17 identified species, 58.8% (10 species) were confirmed via direct field sampling, where a total of 52 specimens were collected and identified. The remaining 41.2% (7 species) were documented through the integration of historical herbarium records and digital databases. Confirmed species include Inga acuminata Benth., Inga cinnamomea Spruce ex Benth., Inga cocleensis Pittier, Inga densiflora Benth., Inga edulis Mart., Inga feuillei DC., Inga insignis Kunth, Inga marginata Kunth, Inga multijuga (Benth.) Kuntze, Inga oerstediana Benth., Inga punctata Willd., Inga sapindoides Willd., Inga silanchensis T.D.Penn., Inga spectabilis (Vahl) Willd., Inga striata Benth., Inga velutina Willd., and Inga vera Willd. Detailed documentation of these sources is provided in Appendix A, and their spatial distribution and morphological characteristics are shown in Figure 2, Figure 3 and Figure A1.

3.2. Thermal and Altitudinal Distribution Patterns

The analysis of the altitudinal distribution reveals two different ecological behaviors among the identified species (Table 2).
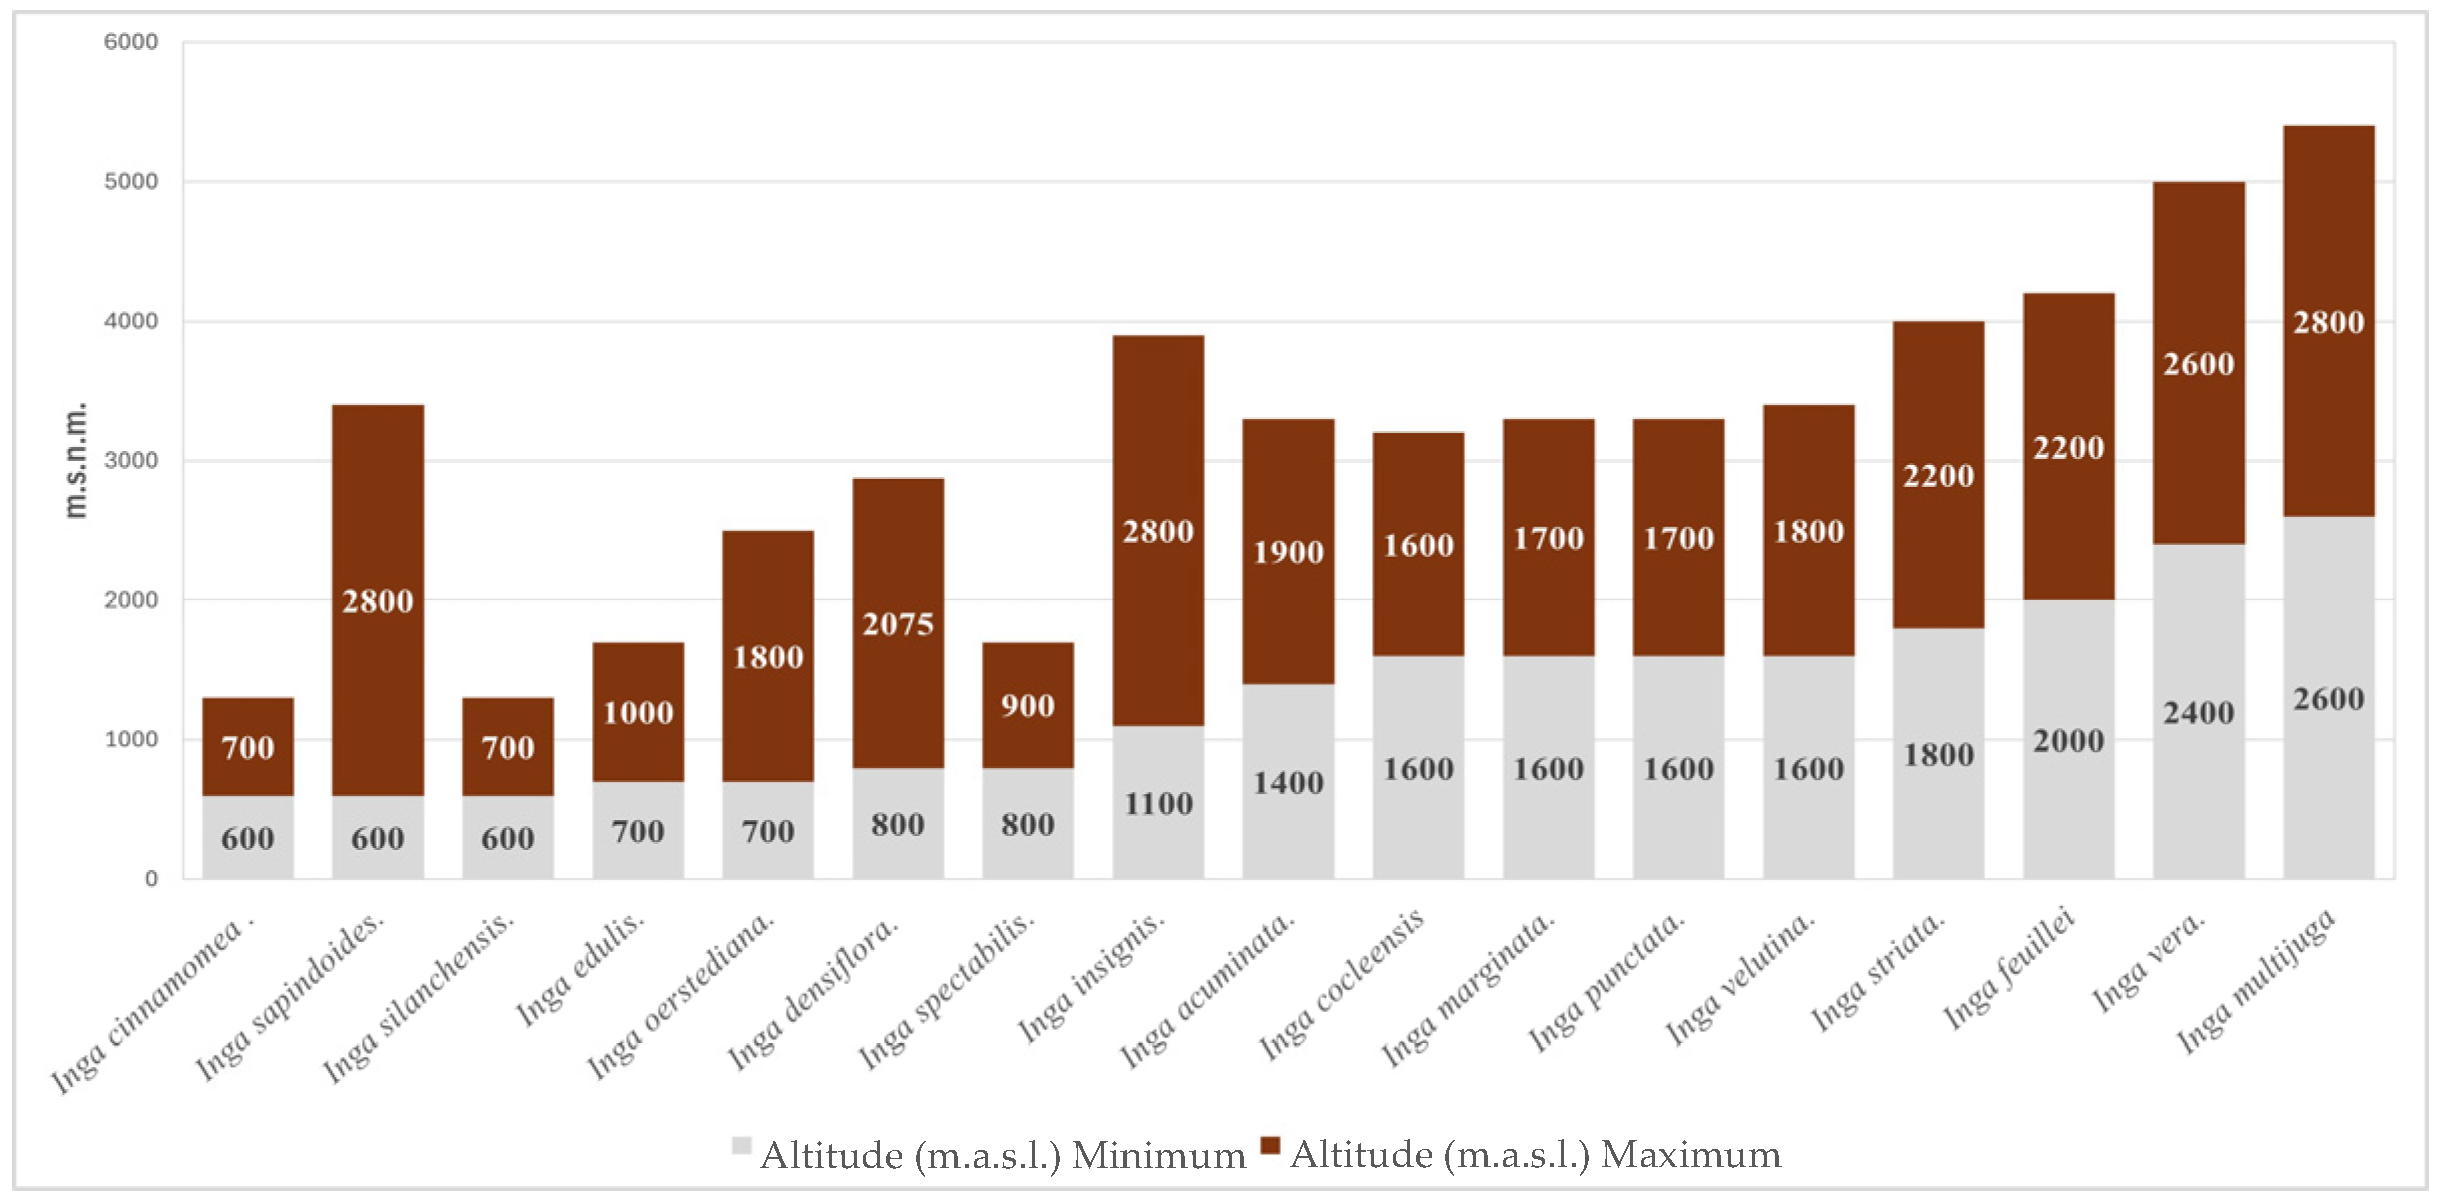
  • Specialized species: A group of species, including I. cinnamomea, I. silanchensis, I. edulis, I. spectabilis, I. marginata, I. punctata, I. velutina and I. feuillei, that occupy narrow altitudinal ranges with variations of less than 500 m. These species are restricted to specific microhabitats (Table 2 and Figure A2 in Appendix B).
  • Generalist species: In contrast, I. sapindoides, I. oerstediana, I. densiflora, I. insignis and I. striata exhibit extensive plasticity and thrive across broad elevation gradients. For example, I. densiflora was recorded between 800 and 2075 m a.s.l., and I. sapindoides between 600 and 2800 m a.s.l. (Table 2 and Figure A2).

Table 2. Edaphoclimatic characteristics of the Inga species in Imbabura *.
SpeciesAltitude (m a.s.l.)Temp. (°C)Precip. (mm)Soil OrderSoil TexturepH
I. edulis700–100021–221500–2000MollisolClay-LoamSlightly Acidic
I. feuillei2000–220015–16500–750MollisolSandy LoamAlkaline
I. multijuga2600–280012–13750–1000InceptisolLoamNeutral
I. marginata1600–170017–191750–3000InceptisolSandy LoamNeutral
I. oerstediana700–180018–232000–2500Incept. + EntisolLoamMed. Acidic
I. insignis1100–280011–21500–1500Incept. + MollisolLoam/SandyVariable
I. sapindoides600–280012–23750–2500InceptisolClay-LoamSlightly Acidic
I. striata1800–220015–17250–1750Incept. + MollisolSandy LoamNeutral
I. silanchensis600–70022–233000–3500InceptisolLoamAcidic
I. spectabilis800–90021–221750–2000MollisolN/AN/A
I. densiflora800–207514–211000–3000Incept. + MollisolClay-SandySlightly Acidic
I. cinnamomea60022–233000–3500InceptisolLoamAcidic
I. vera2400–260013–141250–1500Incept. + EntisolClay-LoamSlightly Acidic
I. cocleensis160017–182500–3000InceptisolSandy LoamNeutral
I. acuminata1400–190016–181750–2000Incept. + EntisolSandy LoamMed. Acidic
I. velutina1600–180017–182500–3000Incept. + EntisolClay-LoamSlightly Acidic
I. punctata1600–170017–182500–3000InceptisolSandy LoamNeutral
Note. * More information in Supplementary Materials. N/A—Not applicable. Bodies of water (lagoons, rivers, channels and meanders, low terraces, swamps, marshes, estuaries, etc.)
Regarding thermal niches, 70.6% of the species (12 species) inhabit areas with narrow thermal fluctuations (average annual variation <2 °C) (Table 2). On the contrary, species such as I. oerstediana and I. insignis tolerate broader thermal ranges (variation from 5 to 11 °C), which correlates with their broader altitudinal distribution (Table 2).

3.3. Soil Preferences and Precipitation Regimes

Among the variables related to soil categories, a marked preference for specific soil conditions is indicated. The distribution of species according to soil order and texture is summarized in Table 2.
  • Soil texture: Species with a textural preference for sandy loam, derived from recent volcanic ash, are I. feuillei, I. marginata and I. punctata, while I. densiflora showed adaptation to sandy clay soils.
  • Soil taxonomy: The genus in Imbabura is mainly associated with Inceptisols and Mollisols. I. edulis and I. striata are notably associated with Mollisols, while I. multijuga and I. silanchensis are restricted to Inceptisols.
  • pH tolerance: Most species (approx. 94%) thrive in neutral to slightly acidic soils (pH ≈ 6.5–7.0). However, I. insignis and I. silanchensis tolerate acidic conditions, while I. feuillei was the only species recorded in alkaline soils.
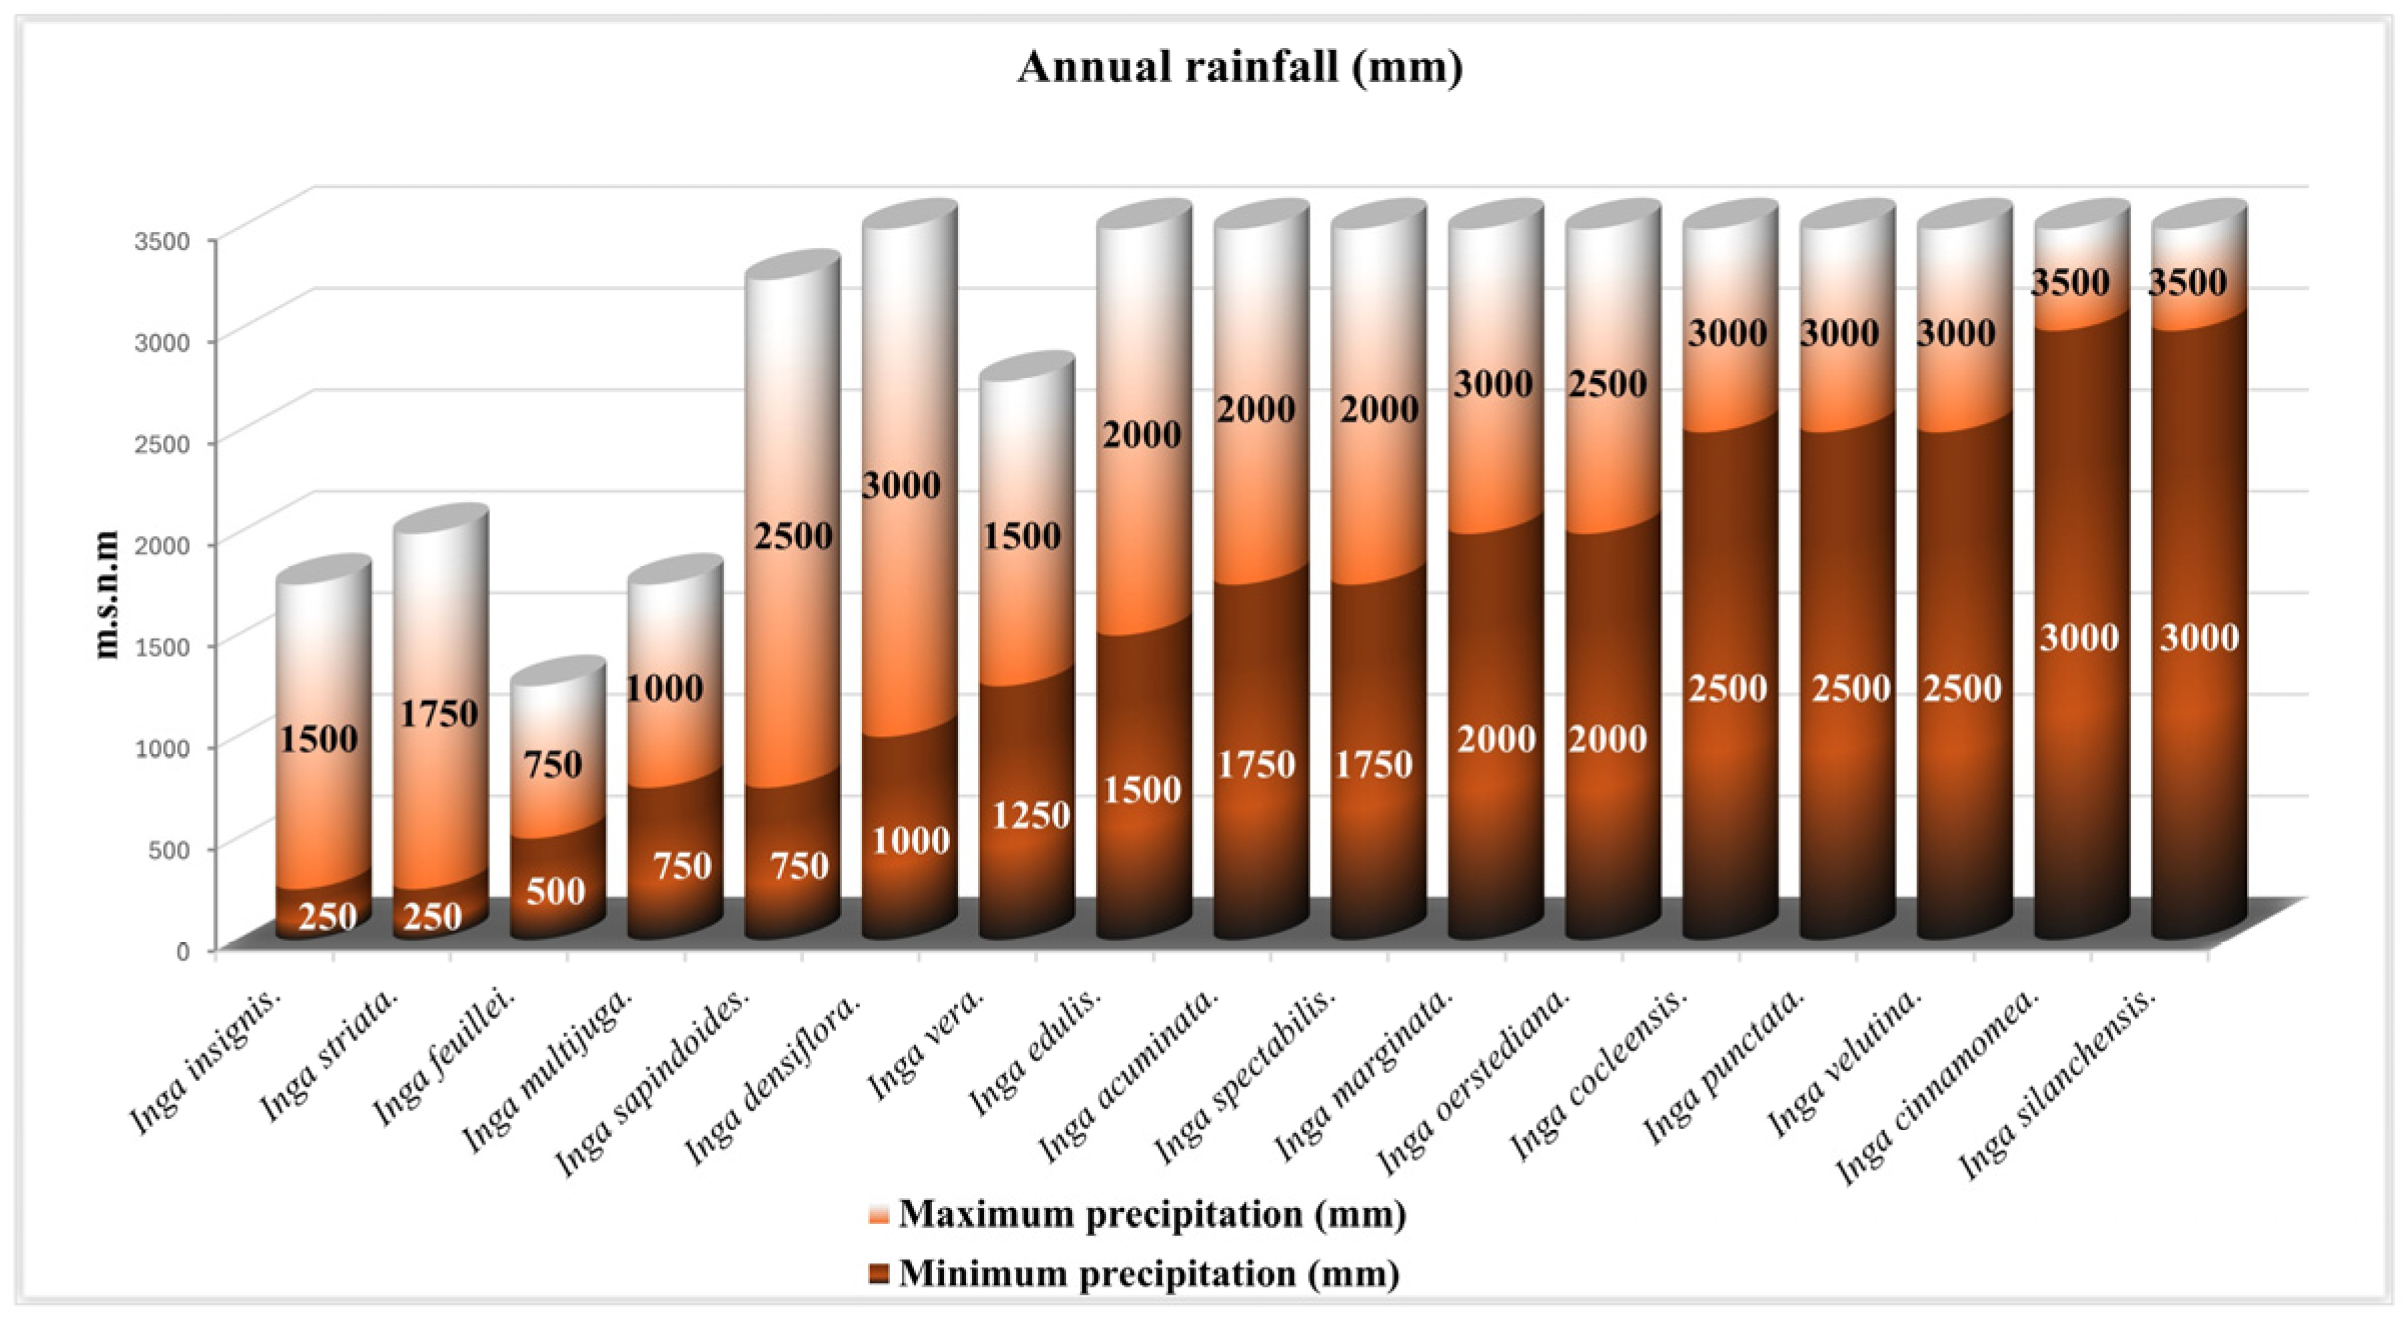
Regarding precipitation, I. feuillei and I. multijuga demonstrate resistance to dry conditions (500–750 mm/year), while most of the genus species requires humid regimes (1250–3000 mm/year) (Figure A3).

4. Discussion

4.1. Ecological Filters: Altitude and Climate Differentiation

The high local richness of Inga spp. recorded in Imbabura (17 species within ~4800 km2) can be framed primarily within the Humboldtian perspective of plant geography, where climatic gradients act as primary ecological filters. We identify two different adaptive strategies:
  • Specialists: A total of 58.8% of the species occupy restricted altitudinal floors. This pattern supports recent findings in Andean tropical forests, where the rate of thermal gradient restricts the distribution of trees to specific thermal floors [20]. These limited-range species are particularly susceptible to biotic attrition driven by climate change [21]. Although sampling along road edges facilitates the recording of species associated with human dispersal, the documented presence of these forest specialists confirms that the assessed corridors retain elements of the forest’s original biodiversity. This observation is crucial, as it demonstrates that, despite anthropogenic disturbances along road edges, these ecosystems still function as refuges for taxa with highly specific niche requirements.
  • Generalists and Distribution Changes: Species such as I. densiflora and I. sapindoides, exhibited extensive ecological plasticity across the Andean gradient. Notably, our data show that I. densiflora reaches 2075 m a.s.l., exceeding the previously reported upper limit of 1900 m for the region [22]. This upward extension could be an indicator of the thermophilization of Andean forests, a process where lowland species migrate upslope in response to increasing temperatures—a phenomenon widely documented in the tropical Andes [23,24,25]. However, while this finding is suggestive, its interpretation as an active upward migration event must be treated with caution due to the lack of direct temporal data in this study. Nonetheless, this record aligns with the elevational migration trends observed in other sectors of the Andes, suggesting that species with high plasticity may be expanding their fundamental niche into higher elevations. Conversely, for less adaptable species, ecotonal barriers could be acting as distribution limits, increasing their vulnerability to climate change and habitat fragmentation [26].

4.2. Edaphic Influence, Nitrogen Fixation and Functional Traits

Edaphic factors play a fundamental role in the distribution of Inga. While traditional literature often describes Inga habitats generally, our study correlates specific species with soil texture and taxonomy (Mollisols/Inceptisols). As nitrogen-fixing legumes, Inga species present a competitive advantage in nitrogen-poor soils [27]; however, its distribution in montane forests could be more strongly limited by soil phosphorus (P) availability or acidity than by nitrogen [28,29,30]. The specificity of I. insignis for acidic soils and of I. feuillei for alkaline conditions supports the habitat-filtering hypothesis. Additionally, the balance between growth and defense is crucial in this genre. Species that invest heavily in chemical defenses (saponins, phenolics) tend to be specialists in resource-poor environments [31,32], while fast-growing generalists may invest less in defense [33,34].

4.3. Geological and Evolutionary Multi-Scale Drivers of Local Inga Richness in Imbabura

Our results suggest that the high diversity of Inga spp. in Imbabura is closely linked to current environmental heterogeneity. Although this study is based on contemporary ecological data, we propose that the geological history of the past 10 million years serves as a relevant interpretive backdrop. DNA sequence data point to recent diversification in Inga, which may have occurred in the past 10 million years, with many species arising as recently as 2 million years ago [35].
This pattern aligns with the late Miocene–Pliocene uplift of the northern Andes, which established steep elevational gradients, reorganized drainage systems, and reshaped precipitation regimes, thereby creating closely juxtaposed montane, cloud forest, and inter-Andean environments over short distances [36,37,38]. Superimposed on this orogenic framework, recurrent Quaternary volcanism in northern Ecuador (e.g., Imbabura, Cotacachi–Cuicocha, Mojanda–Fuya Fuya) generated heterogeneous deposits of tephra and lava, contributing to a spatially complex mosaic of substrates that differ in age, texture, and mineralogical composition. These volcanic inputs not only modified local topography and hydrology, but also drove pedogenesis across contrasting temporal scales, leading to the development of diverse volcanic soils with distinct physical and chemical properties.
Quaternary climatic oscillations subsequently drove repeated upslope and downslope shifts of vegetation belts, modulating population connectivity along elevational gradients and promoting cycles of isolation and secondary contact that may have reinforced lineage divergence [6,35]. Across the tropical Andes, these gradients impose strong thermal and moisture constraints on tree distributions, with specialized communities often exhibiting limited capacity to track climatic warming compared with more generalist assemblages [9,10,39]. In this framework, glacial–interglacial cycles likely functioned as recurrent “connectivity switches” for montane populations: cooler phases displaced forest belts downslope, whereas warmer interglacials promoted upslope expansion and compression of montane habitats [6]. Consequently, the interaction among tectonic uplift, volcanic disturbance, and climatic oscillations has produced a highly heterogeneous landscape in which soil development trajectories—strongly influenced by tephra age and composition—underpin patterns of habitat differentiation and contribute to the remarkable local diversity observed in Andean forest systems.
Repeated upslope and downslope shifts of vegetation belts may have fragmented populations along steep elevational gradients and subsequently reconnected them, potentially increasing genetic structuring and creating opportunities for ecological divergence. Contemporary observations of upslope compositional change (“thermophilization”) and elevational migration of Andean tree species further support the plausibility of strong, elevation-driven demographic dynamics operating on ecological timescales and accumulating over the Quaternary [9,40]. In parallel, Quaternary volcanic activity has likely played a key role in shaping present-day soil heterogeneity through the deposition and reworking of tephra with contrasting ages, textures, and geochemical properties [7,8]. In this context, the coexistence of edaphic specialists (e.g., Inga multijuga and Inga silanchensis, restricted to Inceptisols) is most plausibly explained by the stratification of volcanic ash layers and the resulting variation in soil texture and pH observed in our study, which may promote fine-scale habitat differentiation and niche partitioning along edaphic gradients.
In northern Ecuador, tephrostratigraphic studies indicate that volcanic ash soils commonly comprise multiple discrete tephra layers and exhibit pronounced vertical and lateral variability in their physical and geochemical properties [8]. This heterogeneity is particularly relevant for nutrient dynamics in volcanic and strongly weathered tropical soils, where phosphorus availability and fixation processes can strongly constrain plant distributions [15,22]. Fine-scale edaphic mosaics arising from such variability may therefore promote habitat specialization and local-scale niche partitioning, especially where soil differences interact with biotic pressures such as herbivory [16]. Although our dataset does not include phylogeographic or tephrostratigraphic tests, the observed coexistence of specialist and generalist Inga species across heterogeneous substrates is consistent with long-term landscape renewal driven by volcanic activity and with soil-mediated ecological divergence.
For Inga in Imbabura, the coexistence of narrow-range taxa and broader elevational generalists is consistent with a landscape in which connectivity may have fluctuated repeatedly through time, while dispersal and establishment were likely filtered by both climatic variability and habitat discontinuities [29,30,41]. The high documented species richness of Inga in the province (17 species) is plausibly linked to the combined effects of Andean uplift, persistent Quaternary volcanism, and the resulting edaphoclimatic heterogeneity across short elevational distances [35,42]. In this context, the restriction of species such as Inga multijuga and Inga silanchensis to Inceptisols is consistent with soil-mediated habitat specialization [23,24], and suggests that the physical and geochemical properties associated with relatively young volcanic ash may act as selective filters promoting niche specialization and local-scale coexistence. This interpretation is further supported by evidence of rapid diversification within Inga [35], the role of antiherbivore defenses in shaping ecological differentiation within the genus [21], and the strong influence of phosphorus dynamics in volcanic and highly weathered tropical soils [28].

4.4. Biotic Interactions and Human-Mediated Landscapes

Within this geodynamic context, biotic interactions and anthropogenic landscapes can further shape realized distributions. Inga is well known for strong biotic interactions (e.g., herbivory pressures and defense syndromes), and diversification in the genus has been linked to trait divergence associated with species coexistence and niche differences [5,18,19]. In addition, Neotropical forests are increasingly recognized as historically influenced by human management and landscape domestication, which can alter local abundance patterns and dispersal opportunities for useful taxa [12,17].
Many Inga species (including cultivated or managed forms) are prominent in agroforestry systems, where they provide shade, biomass inputs, and soil fertility services; these systems can act as semi-natural habitat networks that maintain gene flow and facilitate persistence across fragmented landscapes [42,43,44]. The predominance of I. edulis (local name: guaba) in agricultural mosaics in Imbabura confirms its status as a domesticated or semi-domesticated species, widely dispersed by humans for its fruit pulp [34,41,45,46]. This species, along with I. insignis, plays a vital role in local agroforestry systems [47,48]. Unlike wild species confined to forest remnants (I. oerstediana), these “anthropogenic” species benefit from human disturbances [33,46]. Recognizing this dual function—ecological keystones in forests and productive assets on farms—is essential for landscape-scale and biodiversity conservation [28,49]. Therefore, the results obtained reflect the current composition of a landscape where the original biodiversity of the montane forest coexists with species that have been integrated into the agricultural matrix through human intervention.

5. Conclusions

This study increases the documented richness of Inga in Imbabura from six to seventeen species, revealing exceptionally high local diversity within a relatively small but environmentally heterogeneous Andean landscape. The distribution of Inga across the province reflects the interplay of steep elevational gradients, precipitation variability, and edaphic heterogeneity—particularly soil texture and pH—resulting in a discontinuous spatial pattern in which specialist species are restricted to specific microhabitats, while generalists occupy broader environmental ranges.
We interpret this elevated richness as emerging from the combined influence of (i) Miocene–Pliocene Andean uplift, which generated sharp climatic and topographic gradients; (ii) Quaternary climatic oscillations, which may have repeatedly modified elevational connectivity and population structure; and (iii) persistent volcanism, which both reshaped forest structure through disturbance and generated long-term edaphic mosaics via tephra stratification and soil profile complexity. Together, these interacting drivers likely intensified ecological filtering and promoted niche partitioning, consistent with the observed coexistence of elevational and edaphic specialists alongside broad-tolerance generalists within a dynamic, disturbance-influenced landscape.
These findings highlight the vulnerability of specialized populations to habitat fragmentation and climate change. Therefore, conservation strategies must be tailored to protect these critical ecological niches rather than applying generic forest management policies. From a conservation and management perspective, maintaining Inga diversity in Imbabura will likely require protecting elevational corridors and microrefugia across soil mosaics, while also accounting for ongoing climate-driven compositional shifts in Andean forests. Because several Inga species are integral to agroforestry and restoration systems, strengthening landscape connectivity through well-managed shade-tree networks may provide complementary benefits for biodiversity persistence and ecosystem services.
Finally, given the observed presence of domesticated species in agricultural mosaics, future research should integrate ethnobotanical approaches to quantify the role of local human communities in the conservation and dispersal of Inga species in the Andean region.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/f17040508/s1, Table S1: Field verification and samples collection for the UTN herbarium.

Author Contributions

Conceptualization, H.O.P.R.; Methodology, H.O.P.R.; Validation, W.R.F.; Formal Analysis, H.O.P.R. and W.R.F. Research, H.O.P.R.; Resources, H.O.P.R.; Data Curation, H.O.P.R.; Writing—preparation of original draft, H.O.P.R., W.R.F. and E.S.; Writing—Review and Editing, W.R.F. Visualization, H.O.P.R.; Supervision W.R.F. and E.S. All authors have read and agreed to the published version of the manuscript.

Funding

This research did not receive external funding. Logistical and laboratory support were provided by the Technical University of the North (UTN) and the Forest Sciences Research Group (GICFOR); and the publication costs were covered by the Technical University of the North, code: Investiga UTN-2025-1449.

Data Availability Statement

The data presented in this study are available in this article and Supplementary Materials. Publicly available datasets were also analyzed in this study. This data can be found in ref. [12], Herbario UTN: https://www.gbif.org/occurrence/search?publishing_org=e1f3033f-176a-4e5e-8b97-7f1f000fcc2a (accessed 25 May 2025), and Inga data base: https://utneduec-my.sharepoint.com/my?id=%2Fpersonal%2Fhoparedes%5Futn%5Fedu%5Fec%2FDocuments%2FDOCTORADO%2FBase%20de%20datos%20Inga&viewid=a5d71496%2Df78c%2D447b%2Db989%2Df76135e75432 (accessed 5 November 2025). Further inquiries can be directed to the corresponding author.

Acknowledgments

The authors express their gratitude to Nixon Revelo for his motivation and expert guidance. We thank the Technical University of the North (UTN) for allowing us access to the HUTN Herbarium and the Forest Engineering laboratories. The main author appreciates the recognition by SENESCYT as a researcher (Registration No. REGINV-21-05398). This study was carried out under research permit No. MAATE-ARSFC-2023-0036, granted by the Ministry of Environment, Water and Ecological Transition of Ecuador.

Conflicts of Interest

The authors declare no conflicts of interest.

Appendix A. Herbariums Reviewed in Their Databases and Contained Information on the Genus Inga in Imbabura

I. cocleensis: 11 August 1990; Rubio and Quelal (1); 604 (MO); I. densiflora: 11 August 1990 and 15 June 2025; Rubio, Quelal, Vargas, Defas and Reyes (2); 563 and 6284 (MO; QCNE); I. feuillei: 1988; Madsen (1); 84308 (AAU); I. insignis: 15 August 1949, 3 November 1986, 18 April 1988, 21 April 1993 and 8 March 2002; Jaramillo, Caranqui, Acosta Solís, Pennington, Vargas and Zak (5); 577, 13869, 3655, 9244 and 13368 (F, MO, QCNE); I. marginata: 15 January 1992 and 31 May 2009; Tipaz, Quelal, Edwards and Palacios (2); 608 and 16792 (MO, QCNE); I. multijuga: 14 May 2009; Palacios (1); 16736 (QCNE), I. oerstediana: 1992 and 15 March 2012; Medina, Cardona, Rojas, Viancha, Vega, Prieto, Herrera and Pennington (4); 13967, 11966, 11965 and 11964 (MO); I. punctata: 11 August 1990; Rubio and Quelal (1); 579 (MO); I. sapindoides: 30 May 1949; Acosta Solís (1); 12637 (F); I. striata: 8 December 1990 and 14 January 1991; Cerón, Montesdeoca and Palacios (2); 12576 and 6797 (MO); I. velutina: 27 October 2005; Vargas, Defas and Reyes (1); 6290 (QCNE), I. vera: 18 February 2007; Palacios (1); 17536 (MO).
  • QCNE—National Biodiversity Institute of Ecuador
  • MO—Tropics
  • AAU—Aarhus University Herbarium
  • F—SQF Herbarium

Appendix B

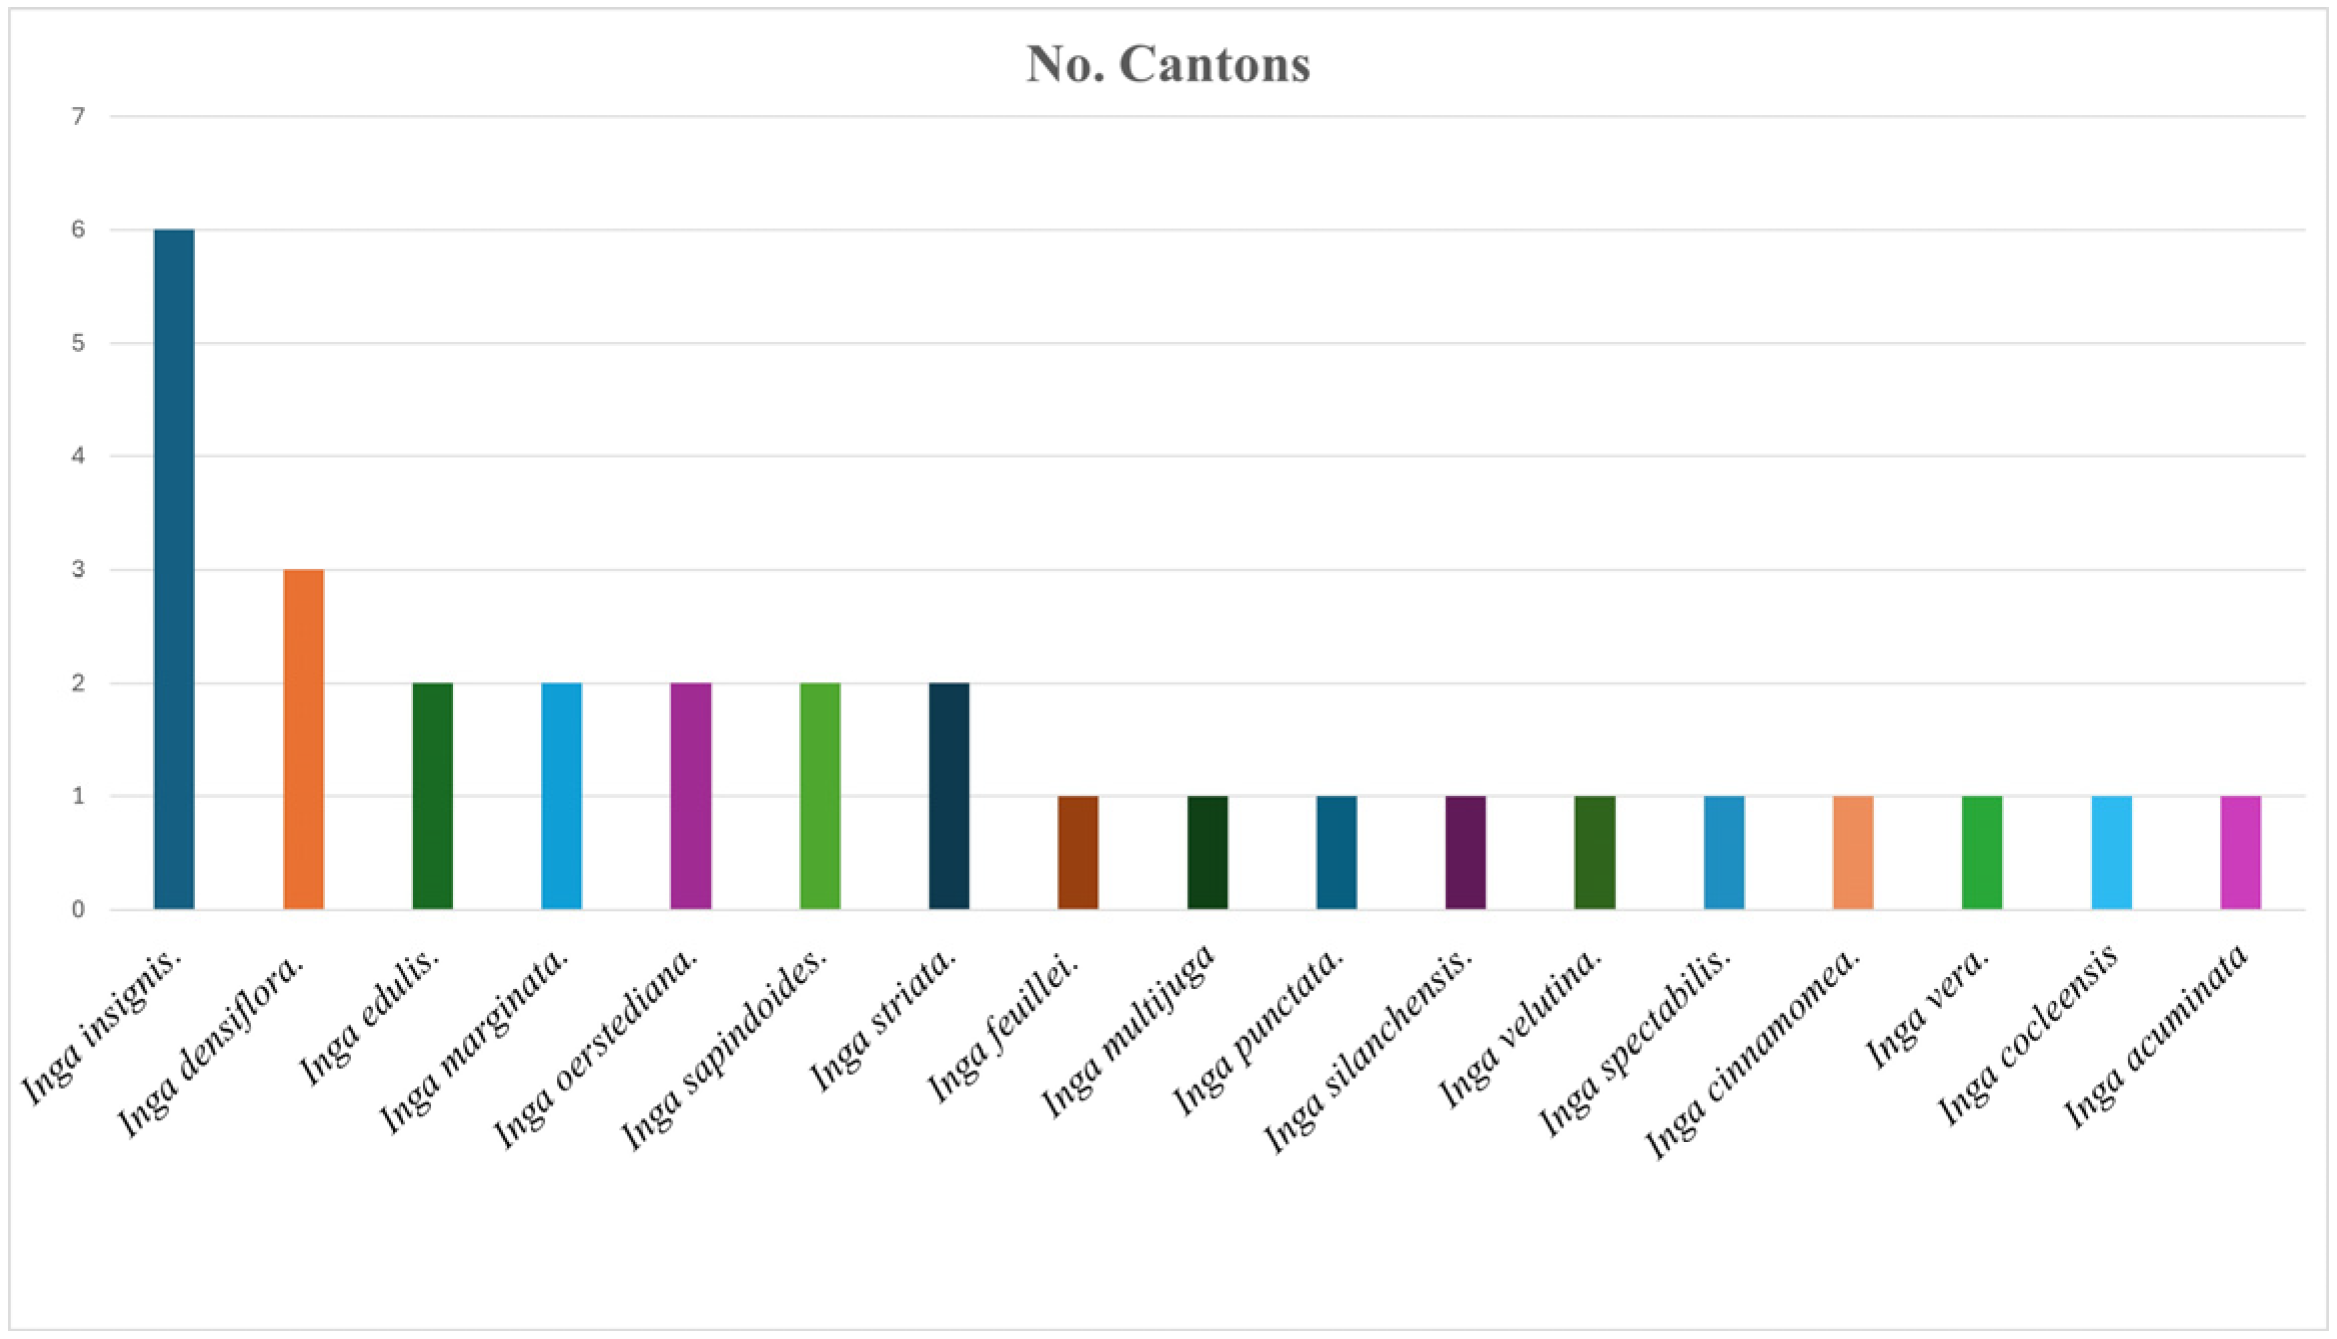
Figure A1. Species of the genus Inga in the cantons of Imbabura.
Forests 17 00508 g0a1
Figure A2. Distribution ranges of species of the genus Inga in Imbabura.
Forests 17 00508 g0a2
Figure A3. Precipitation ranges of species of the genus Inga in Imbabura.
Forests 17 00508 g0a3

References

  1. Tomaseili, M. Introducción a la dendrocronología: Anatomía de la madera en los trópicos. In Proceedings of the II Curso Internacional: Anatomía y Dendrocronología Tropical, Huancayo, Peru, 6–10 November 2023; p. 5. [Google Scholar]
  2. Neill, D. La evolución de las especies en el Ecuador: Las Magnoliaceae. In Proceedings of the V Congreso de Bosques de la Amazonía Ecuatoriana; Universidad Estatal Amazónica: Puyo, Ecuador, 2019; p. 5. [Google Scholar]
  3. Ministerio del Ambiente del Ecuador (MAE). Deforestación del Ecuador Continental 2014–2016; Ministerio del Ambiente del Ecuador (MAE): Quito, Ecuador, 2017. [Google Scholar]
  4. Global Forest Watch. Dashboard de Imbabura, Ecuador. Available online: https://www.globalforestwatch.org/dashboards/country/ECU/11/ (accessed on 16 March 2026).
  5. Bruneau, A.; de Queiroz, L.P.; Ringelberg, J.; Borges, L. Advances in Legume Systematics 14. Classification of Caesalpinioideae. Part 2: Higher-level classification. PhytoKeys 2024, 239, 1–552. [Google Scholar] [CrossRef] [Scilit]
  6. Palacios, W. Árboles del Ecuador: Familias y Géneros; Universidad Técnica del Norte: Ibarra, Ecuador, 2016. [Google Scholar]
  7. Pennington, T.D.; Revelo, N. El Género Inga en el Ecuador: Morfología, Distribución y Usos; Herbario Nacional del Ecuador: Quito, Ecuador, 1997. [Google Scholar]
  8. Gutiérrez, E. Efecto del cambio climático en la distribución potencial de cinco especies arbóreas de bosque templado en México. Rev. Mex. Biodivers. 2014, 85, 52–55. [Google Scholar] [CrossRef] [Scilit]
  9. Denevan, W.M. The Pristine Myth: The Landscape of the Americas in 1492. Ann. Assoc. Am. Geogr. 1992, 82, 369–385. [Google Scholar] [CrossRef] [Scilit]
  10. Sánchez-Albornoz, N. The Population of Latin America: A History; University of California Press: Berkeley, CA, USA, 1984. [Google Scholar]
  11. KoboToolbox. Available online: https://www.kobotoolbox.org/ (accessed on 23 January 2026).
  12. Inga Mill. in GBIF Secretariat. 2023. Available online: https://www.gbif.org/species/2965936 (accessed on 28 August 2023).
  13. GBIF. Género Inga en Imbabura. Available online: https://www.gbif.org/occurrence/download/0019257-250310093411724 (accessed on 20 March 2025).
  14. Ministerio de Ambiente, Agua y Transición Ecológica del Ecuador (MAATE). Permiso de Investigación No. MAATE-ARSFC-2023-0036; Ministerio de Ambiente, Agua y Transición Ecológica del Ecuador (MAATE): Quito, Ecuador, 2023. [Google Scholar]
  15. Pennington, T.D. Flora ilustrada peruana—Inga (Leguminosas): Guabas y pacáes del Perú. Rev. For. Perú 2024, 39, 5–453. [Google Scholar] [CrossRef] [Scilit]
  16. Instituto Nacional de Estadística y Censos (INEC). Límites Provinciales y Cantonales; Instituto Nacional de Estadística y Censos (INEC): Quito, Ecuador, 2024. [Google Scholar]
  17. National Institute of Meteorology and Hydrology (INAMHI). Visor Climático. Available online: http://www.inamhi.gob.ec/visor/ (accessed on 20 April 2025).
  18. Ministerio de Agricultura, Ganadería, Acuacultura y Pesca (MAGAP). Mapa de Fertilidad de Suelos del Ecuador; Jiménez, J., Ed.; Ministerio de Agricultura, Ganadería, Acuacultura y Pesca (MAGAP): Quito, Ecuador, 2012. [Google Scholar]
  19. Ministerio de Ambiente, Agua y Transición Ecológica del Ecuador (MAATE). Mapa Interactivo del Ecuador. Available online: http://ide.ambiente.gob.ec/mapainteractivo/ (accessed on 10 January 2025).
  20. Holl, K.D.; Aide, T.M. When and where to actively restore ecosystems? For. Ecol. Manag. 2011, 261, 1558–1563. [Google Scholar] [CrossRef] [Scilit]
  21. Kursar, T.A.; Dexter, K.G.; Lokvam, J.; Pennington, R.T.; Richardson, J.E.; Weber, M.G.; Murakami, E.T.; Drake, S.T.; McGregor, R.; Coley, P.D. The evolution of antiherbivore defenses and their role in binary risk of herbivory in Inga. Proc. Natl. Acad. Sci. USA 2009, 106, 18073–18078. [Google Scholar] [CrossRef] [Scilit]
  22. Paredes, H. KoBoToolbox. Available online: https://kf.kobotoolbox.org/#/projects/home (accessed on 4 May 2024).
  23. Dexter, K.G.; Terborgh, J.W.; Cunningham, C.W. Convergence in habitat specialization in Inga (Fabaceae). Syst. Biodivers. 2012, 10, 235–244. [Google Scholar]
  24. Dexter, K.G.; Chave, J. Evolutionary patterns of range size, niche breadth and species survival in Inga. J. Biogeogr. 2010, 37, 2011–2020. [Google Scholar]
  25. Duque, A.; Stevenson, P.R.; Feeley, K.J. Thermophilization of adult and juvenile tree communities in the northern Tropical Andes. Proc. Natl. Acad. Sci. USA 2015, 112, 10744–10749. [Google Scholar] [CrossRef] [Scilit]
  26. Schley, R.J.; de la Estrella, M.; Pérez-Escobar, O.A.; Bruneau, A.; Barraclough, T.G.; Forest, F.; Klitgård, B.B. TThe genome sequence of Inga oerstediana Benth. Wellcome Open Res. 2024, 9, 607. [Google Scholar] [CrossRef] [Scilit]
  27. Nichols, J.D.; Carpenter, F.L. Interplanting Inga edulis with Terminalia amazonia in Costa Rica. Agrofor. Syst. 2006, 66, 1–7. [Google Scholar]
  28. Vitousek, P.M.; Porder, S.; Houlton, B.Z.; Chadwick, O.A. Terrestrial phosphorus cycling: Regional variations and global disparities. Biogeochemistry 2010, 100, 227–239. [Google Scholar]
  29. Colwell, R.K.; Brehm, G.; Cardelús, C.L.; Gilman, A.C.; Longino, J.T. Global warming, elevational range shifts, and lowland biotic attrition. Science 2008, 322, 258–261. [Google Scholar] [CrossRef] [Scilit]
  30. Feeley, K.J.; Silman, M.R.; Bush, M.B.; Farfan, W.; Garcia, K.G.; Malhi, Y.; Meir, P.; Revilla, N.S.; Quispe, M.N.R.; Miles, L. Upslope migration of Andean trees. J. Biogeogr. 2011, 38, 783–791. [Google Scholar] [CrossRef] [Scilit]
  31. Coley, P.D.; Lokvam, J.; Rudolph, K.; Pruitt, K.; Seger, J.; Kursar, T.A. Divergent defensive strategies of young leaves in two species of Inga. Ecology 2005, 86, 2633–2643. [Google Scholar] [CrossRef] [Scilit]
  32. Endara, M.J.; Weinhold, A.; Cox, J.E.; Wiggins, N.L.; Coley, P.D.; Kursar, T.A. Coevolutionary arms race versus host defense chase in a tropical herbivore–plant system. Proc. Natl. Acad. Sci. USA 2015, 112, E4569–E4576. [Google Scholar] [CrossRef] [Scilit]
  33. Clement, C.R. 1492 and the loss of Amazonian crop genetic resources. I. The relation between domestication and population decline. Econ. Bot. 1999, 53, 188–202. [Google Scholar] [CrossRef] [Scilit]
  34. Lojka, B.; Dumas, L.; Preininger, D.; Polesny, Z.; Banout, J. The use and integration of Inga edulis in agroforestry systems in the Peruvian Amazon. Agrofor. Syst. 2011, 83, 67–81. [Google Scholar]
  35. Richardson, J.E.; Pennington, R.T.; Pennington, T.D.; Hollingsworth, P.M. Rapid diversification of a species-rich genus of neotropical rain forest trees. Science 2001, 293, 2242–2246. [Google Scholar] [CrossRef] [Scilit]
  36. Antonelli, A.; Nylander, J.A.A.; Persson, C.; Sanmartín, I. Tracing the impact of Andean uplift on Neotropical plant evolution. Proc. Natl. Acad. Sci. USA 2009, 106, 9749–9754. [Google Scholar] [CrossRef] [Scilit]
  37. Hoorn, C.; Wesselingh, F.P.; Ter Steege, H.; Bermudez, M.A.; Mora, A.; Sevink, J.; Sanmartín, I.; Sanchez-Meseguer, A.; Anderson, C.L.; Figueiredo, J.P.; et al. Amazonia through time: Andean uplift, climate change, and biodiversity. Science 2010, 330, 927–931. [Google Scholar] [CrossRef] [Scilit]
  38. Hall, M.L.; Mothes, P. Volcanic history of the Ecuadorian Andes. J. Volcanol. Geotherm. Res. 2008, 176, 1–17. [Google Scholar] [CrossRef] [Scilit]
  39. Robin, C.; Samaniego, P.; Le Pennec, J.L.; Mothes, P.; van der Plicht, J.; Albarede, F.; Hall, M.L.; Monzier, M.; Eissen, J.P.; Fornari, M. Late Pleistocene volcanic activity in northern Ecuador. Bull. Volcanol. 2009, 71, 1043–1061. [Google Scholar]
  40. Paredes, H.; Rosales, O.; Varela, G.; Carvajal, G.; León, M. Herbario Universidad Técnica del Norte (HUTN), un laboratorio para conocer la diversidad de especies forestales del Ecuador. Cienc. Lat. 2023, 7, 1167–1184. [Google Scholar] [CrossRef] [Scilit]
  41. Fadrique, B.; Homeier, J.; Baez, S.; Duque, A.; Tello, J.S.; Renner, S.S.; Feeley, K.J. Widespread but heterogeneous responses of Andean forests to climate change. Nature 2018, 564, 407–411. [Google Scholar] [CrossRef] [Scilit]
  42. Murga, H.; Coronado, M.F.; Abanto-Rodríguez, C.; De Almeida-Lobo, F. Gradiente altitudinal y su influencia en las características edafoclimáticas de los bosques tropicales. Madera Bosques 2021, 27, e271211. [Google Scholar]
  43. Castro, A. Biogeografía y Modelos de Distribución de Especies. WorldClim 2020. Available online: https://www.researchgate.net/publication/344310835_Biogeografia_y_modelos_de_distribucion_de_especies (accessed on 23 October 2025).
  44. Maciel, E.A.; Oliveira-Filho, A.T.; Eisenlohr, P.V. Distribution of Inga species in South America. J. Biogeogr. 2015, 42, 1–12. [Google Scholar]
  45. Lutz, D.A.; Powell, R.L.; Silman, M.R. Andean timberline migration and biodiversity loss with optimization of land management. PLoS ONE 2013, 8, e76101. [Google Scholar] [CrossRef] [Scilit]
  46. Beer, J.; Muschler, R.; Kass, D.; Somarriba, E. Shade management in coffee and cacao plantations. Agrofor. Syst. 1998, 38, 139–164. [Google Scholar] [CrossRef] [Scilit]
  47. Gehring, C.; Vlek, P.L.G.; de Souza, L.A.G.; Denich, M. Biological nitrogen fixation in secondary regrowth in the central Amazon. Agric. Ecosyst. Environ. 2005, 111, 239–252. [Google Scholar] [CrossRef] [Scilit]
  48. Condit, R.; Engelbrecht, B.M.J.; Pino, D.; Pérez, R.; Turner, B.L. Species distributions in response to individual soil nutrients and seasonal drought across a tropical forest landscape. Proc. Natl. Acad. Sci. USA 2013, 110, 5064–5068. [Google Scholar] [CrossRef] [Scilit]
  49. Somarriba, E.; Harvey, C.A.; Samper, M.; Anthony, F.; González, J.; Staver, C.; Rice, R.A. Biodiversity conservation in neotropical coffee (Coffea arabica) plantations. In Agroforestry and Biodiversity Conservation in Tropical Landscapes; Schroth, G., Ed.; Island Press: Washington, DC, USA, 2004; pp. 198–226. [Google Scholar]
Figure 1. Sampling areas in the province of Imbabura.
Forests 17 00508 g001
Figure 2. Species of the genus Inga in Imbabura.
Forests 17 00508 g002
Figure 3. Photographs of fruits from the Inga species: (A) I. acuminata, (B) I. sapindoides, (C) I. edulis, (D) I. vera, (E) I. feuillei, (F) I. multijuga, (G) I. marginata, (H) I. punctata, (I) I. oerstediana, (J) I. insignis, (K) I. striata, (L) I. silanchensis, (M) I. velutina, (N) I. spectabilis, (O) I. densiflora, (P) I. cinnamomea, and (Q) I. cocleensis.
Forests 17 00508 g003
Table 1. Summary of environmental variables, data sources, and spatial resolutions used in the study.
VariableData SourceFormatResolution/Scale
Climate (Bio 1–19) WorldClim 2.1Raster30 arc-sec (1 km2)
Topography (Elevation, TRI, Slope)ALOS PALSARRaster12.5 m
Global Soils (Nitrogen, pH, Texture)SoilGrids 2.0Raster250 m
National Geopedology (Order, Geology)SIGTIERRASPolygon1:25,000
Vegetation CoverMAATEPolygon1:100,000
Note. TRI: Terrain Ruggedness Index; ALOS PALSAR: Advanced Land Observing Satellite Phased Array type L-band Synthetic Aperture Radar; SIGTIERRAS: National System of Information and Management of Rural Lands and Technological Infrastructure; MAATE: Ministry of Environment, Water and Ecological Transition of Ecuador.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.