


Bioactive Constituents, Mechanisms, and Complementary Therapeutic Applications of Food–Medicine Continuum Materia Medica for Atherosclerosis Prevention and Treatment

Abstract
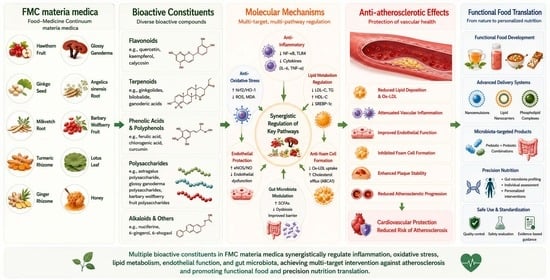
1. Introduction
2. Methodology
3. Bioactive Components of Food and Medicine Continuum Materia Medica
3.1. Flavonoid Compounds
3.2. Terpenoid Compounds
3.3. Polysaccharide Compounds
3.4. Phenolic Acid and Gingerol Compounds
3.5. Other Bioactive Components
4. Anti-Atherosclerotic Molecular Mechanisms
4.1. Improving Endothelial Dysfunction
4.2. Regulating Lipid Metabolism
4.3. Inhibiting Vascular Inflammation
4.4. Anti-Oxidative Stress
4.5. Inhibiting Foam Cell Formation
4.6. Maintaining Plaque Stability
4.7. Regulating the Gut Microbiota–Metabolite–Cardiovascular Axis
4.8. Network Regulatory Mechanisms of Multi-Component Synergy
4.8.1. Component Synergy Within the Same Herb
4.8.2. Comparison with Single-Target Western Medicine Treatment
5. Preventive Applications: From Traditional Medicinal Cuisine to Functional Foods
5.1. Modernization of Traditional Medicinal Cuisine
5.2. Clinical Evidence for Standardized Extracts
5.3. Functional Food Development
5.4. Safety Management and Drug Interactions
6. Summary and Outlook
Author Contributions
Funding
Institutional Review Board Statement
Informed Consent Statement
Data Availability Statement
Acknowledgments
Conflicts of Interest
Abbreviations
| CVD | Cardiovascular disease |
| AS | Atherosclerosis |
| FMC | Food and medicine continuum |
| TCM | Traditional Chinese medicine |
| AMPK | Adenosine 5′-monophosphate-activated protein kinase |
| SREBP-1c | Sterol regulatory element-binding protein-1c |
| PPARα | Peroxisome proliferator-activated receptor alpha |
| PAF | Platelet-activating factor |
| Nrf2 | Nuclear factor erythroid 2-related factor 2 |
| PI3K | Phosphatidylinositol 3-kinase |
| Akt | Protein kinase B |
| eNOS | Endothelial nitric oxide synthase |
| HMG-CoA | 3-hydroxy-3-methylglutaryl-coenzyme A |
| NF-κB | Nuclear factor kappa-light-chain-enhancer of activated B cells |
| MAPK | Mitogen-activated protein kinase |
| HO-1 | Heme oxygenase-1 |
| NQO1 | NAD(P)H quinone oxidoreductase 1 |
| RG-I | Rhamnogalacturonan-I |
| COX | Cyclooxygenase |
| TXA2 | Thromboxane A2 |
| NO | Nitric oxide |
| iNOS | Inducible nitric oxide synthase |
| ARE | Antioxidant response element |
| LDL | Low-density lipoprotein |
| TLR4 | Toll-like receptor 4 |
| TNF-α | Tumor necrosis factor-alpha |
| ICAM-1 | Intercellular adhesion molecule-1 |
| VCAM-1 | Vascular cell adhesion molecule-1 |
| NADPH | Nicotinamide adenine dinucleotide phosphate |
| ROS | Reactive oxygen species |
| LOX-1 | Lectin-like oxidized low-density lipoprotein receptor-1 |
| LDLR | Low-density lipoprotein receptor |
| LXRα | Liver X receptor alpha |
| CYP7A1 | Cytochrome P450 family 7 subfamily A member 1 |
| SCAP | SREBP cleavage-activating protein |
| RCT | Reverse cholesterol transport |
| ABCA1 | ATP-binding cassette transporter A1 |
| HDL | High-density lipoprotein |
| IL-1β | Interleukin-1 beta |
| NLRP3 | NLR family pyrin domain containing 3 |
| MMP | Matrix metalloproteinase |
| TMAO | Trimethylamine N-oxide |
References
- Stark, B.A.; DeCleene, N.K.; Desai, E.C.; Hsu, J.M.; Johnson, C.O.; Lara-Castor, L.; LeGrand, K.E.; A, B.; Aalipour, M.A.; Aalruz, H.; et al. Global, Regional, and National Burden of Cardiovascular Diseases and Risk Factors in 204 Countries and Territories, 1990–2023. J. Am. Coll. Cardiol. 2025, 86, 2167–2243. [Google Scholar] [CrossRef] [Scilit]
- Libby, P.; Buring, J.E.; Badimon, L.; Hansson, G.K.; Deanfield, J.; Bittencourt, M.S.; Tokgözoğlu, L.; Lewis, E.F. Atherosclerosis. Nat. Rev. Dis. Primers 2019, 5, 56. [Google Scholar] [CrossRef] [Scilit]
- Blumenthal, R.S.; Morris, P.B.; Gaudino, M.; Johnson, H.M.; Anderson, T.S.; Bittner, V.A.; Blankstein, R.; Brewer, L.C.; Cho, L.; de Ferranti, S.D.; et al. 2026 ACC/AHA/AACVPR/ABC/ACPM/ADA/AGS/APhA/ASPC/NLA/PCNA Guideline on the Management of Dyslipidemia: A Report of the American College of Cardiology/American Heart Association Joint Committee on Clinical Practice Guidelines. Circulation 2026, 153, e1154–e1276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Imran, T.F.; Khan, A.A.; Has, P.; Jacobson, A.; Bogin, S.; Khalid, M.; Khan, A.; Kim, S.; Erqou, S.; Choudhary, G.; et al. Proprotein convertase subtilisn/kexin type 9 inhibitors and small interfering RNA therapy for cardiovascular risk reduction: A systematic review and meta-analysis. PLoS ONE 2023, 18, e0295359. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- American Diabetes Association Professional Practice Committee for Diabetes. 10. Cardiovascular Disease and Risk Management: Standards of Care in Diabetes—2026. Diabetes Care 2026, 49, S216–S245. [Google Scholar] [CrossRef] [Scilit]
- Banach, M.; Patti, A.M.; Giglio, R.V.; Cicero, A.F.G.; Atanasov, A.G.; Bajraktari, G.; Bruckert, E.; Descamps, O.; Djuric, D.M.; Ezhov, M.; et al. The Role of Nutraceuticals in Statin Intolerant Patients. J. Am. Coll. Cardiol. 2018, 72, 96–118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Collins, R.; Reith, C.; Emberson, J.; Armitage, J.; Baigent, C.; Blackwell, L.; Blumenthal, R.; Danesh, J.; Smith, G.D.; DeMets, D.; et al. Interpretation of the evidence for the efficacy and safety of statin therapy. Lancet 2016, 388, 2532–2561. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Riccardi, G.; Giosuè, A.; Calabrese, I.; Vaccaro, O. Dietary recommendations for prevention of atherosclerosis. Cardiovasc. Res. 2022, 118, 1188–1204. [Google Scholar] [CrossRef] [Scilit]
- Marques-Vidal, P.; Tsampasian, V.; Cassidy, A.; Biondi-Zoccai, G.; Chrysohoou, C.; Koskinas, K.; Verschuren, W.M.M.; Czapla, M.; Kavousi, M.; Kouvari, M.; et al. Diet and nutrition in cardiovascular disease prevention: A scientific statement of the European Association of Preventive Cardiology and the Association of Cardiovascular Nursing & Allied Professions of the European Society of Cardiology. Eur. J. Prev. Cardiol. 2025, 32, 1540–1552. [Google Scholar] [CrossRef] [Scilit]
- Law, S.K.; Au, D.C.T. A review of medicine and food homology on traditional Chinese medicine as functional food. Food Med. Homol. 2026, 3, 9420091. [Google Scholar] [CrossRef] [Scilit]
- Qu, S.; Yu, S.; Ma, X.; Wang, R. “Medicine food homology” plants promote periodontal health: Antimicrobial, anti-inflammatory, and inhibition of bone resorption. Front. Nutr. 2023, 10, 1193289. [Google Scholar] [CrossRef] [Scilit]
- Hou, Y.; Jiang, J.G. Origin and concept of medicine food homology and its application in modern functional foods. Food Funct. 2013, 4, 1727–1741. [Google Scholar] [CrossRef] [Scilit]
- Lyu, C.G.; Kang, C.Z.; Yang, J.; Wang, S.; Wang, R.S.; Wan, X.F.; Guo, L.P. Problems and strategy of further development of Chinese medicinal materials with edible values. Zhongguo Zhong Yao Za Zhi 2022, 47, 6810–6816. [Google Scholar] [CrossRef] [Scilit]
- Downer, S.; Berkowitz, S.A.; Harlan, T.S.; Olstad, D.L.; Mozaffarian, D. Food is medicine: Actions to integrate food and nutrition into healthcare. BMJ 2020, 369, m2482. [Google Scholar] [CrossRef] [Scilit]
- Zhou, D.D.; Luo, M.; Shang, A.; Mao, Q.Q.; Li, B.Y.; Gan, R.Y.; Li, H.B. Antioxidant Food Components for the Prevention and Treatment of Cardiovascular Diseases: Effects, Mechanisms, and Clinical Studies. Oxidaxive Med. Cell. Longev. 2021, 2021, 6627355. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zarenezhad, E.; Hadi, A.T.; Nournia, E.; Rostamnia, S.; Ghasemian, A. A Comprehensive Review on Potential In Silico Screened Herbal Bioactive Compounds and Host Targets in the Cardiovascular Disease Therapy. Biomed. Res. Int. 2024, 2024, 2023620. [Google Scholar] [CrossRef] [Scilit]
- Yamagata, K. Polyphenols Regulate Endothelial Functions and Reduce the Risk of Cardiovascular Disease. Curr. Pharm. Des. 2019, 25, 2443–2458. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sánchez, M.; Romero, M.; Gómez-Guzmán, M.; Tamargo, J.; Pérez-Vizcaino, F.; Duarte, J. Cardiovascular Effects of Flavonoids. Curr. Med. Chem. 2019, 26, 6991–7034. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Garcia, C.; Blesso, C.N. Antioxidant properties of anthocyanins and their mechanism of action in atherosclerosis. Free Radic. Biol. Med. 2021, 172, 152–166. [Google Scholar] [CrossRef] [Scilit]
- Rodriguez-Mateos, A.; Le Sayec, M.; Cheok, A. Dietary (poly)phenols and cardiometabolic health: From antioxidants to modulators of the gut microbiota. Proc. Nutr. Soc. 2025, 84, 279–289. [Google Scholar] [CrossRef] [Scilit]
- Oak, M.H.; Auger, C.; Belcastro, E.; Park, S.H.; Lee, H.H.; Schini-Kerth, V.B. Potential mechanisms underlying cardiovascular protection by polyphenols: Role of the endothelium. Free Radic. Biol. Med. 2018, 122, 161–170. [Google Scholar] [CrossRef] [Scilit]
- Guo, S.; Qiu, S.; Cai, Y.; Wang, Z.; Yang, Q.; Tang, S.; Xie, Y.; Zhang, A. Mass spectrometry-based metabolomics for discovering active ingredients and exploring action mechanism of herbal medicine. Front. Chem. 2023, 11, 1142287. [Google Scholar] [CrossRef] [Scilit]
- Sharma, B.; Yadav, D.K. Metabolomics and Network Pharmacology in the Exploration of the Multi-Targeted Therapeutic Approach of Traditional Medicinal Plants. Plants 2022, 11, 3243. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Li, X.; Wang, L.; Hou, Y.; Liu, Y.; Mao, J.; Zhang, L.; Li, X. Advancing Traditional Chinese Medicine Research through Network Pharmacology: Strategies for Target Identification, Mechanism Elucidation and Innovative Therapeutic Applications. Am. J. Chin. Med. 2025, 53, 2021–2042. [Google Scholar] [CrossRef] [Scilit]
- Wang, Z.; Li, Y.; Yu, P.; Guo, Z.; Huang, X.; Ma, C.; Dong, L.; Luo, P.; Wang, G.; Hu, X.; et al. Research Progress on The Chemical Composition And Pharmacological Effects of Hawthron (Crataegus spp.): A Review. J. Agric. Food Chem. 2026, 74, 145–170. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Liang, R.; Wang, L.; Yan, R.; Hou, R.; Gao, S.; Yang, B. Effects of an aqueous extract of Crataegus pinnatifida Bge. var. major N.E.Br. fruit on experimental atherosclerosis in rats. J. Ethnopharmacol. 2013, 148, 563–569. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, L.; Lu, Z.; Ma, Y.; Cui, P.; Zhang, X.; Gan, J.; Li, G. Hawthorn total flavonoids ameliorate hyperlipidemia through AMPK/SREBP1-c and PPARα/PGC-1α/CPT-1A pathway activation and gut microbiota modulation. J. Sci. Food Agric. 2025, 105, 4326–4337. [Google Scholar] [CrossRef] [Scilit]
- Li, M.; Si, J.Y.; Xie, P.F.; Feng, Z.J.; Li, S.J.; Zhou, F.; Li, J.M. Procyanidin C1 from hawthorn modulates metabolic-inflammatory axis to combat vascular senescence in atherosclerosis. Food Res. Int. 2026, 227, 118224. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jia, H.; Wei, W.X.; Jiang, P.P.; Yu, W.W. Variation in seed quality among Ginkgo biloba L. individuals and selection of superior nut-producing tree. Plant Sci. J. 2025, 43, 770–780. [Google Scholar]
- Shan, S.J.; Shi, L.L.; Liu, C.C.; Jiang, Y.R.; Chen, G.R. Study on Chemical Constituents of n-Butanol Extract of Ginkgo Biloba Seeds. Liaoning Chem. Ind. 2023, 52, 798–800+804. [Google Scholar] [CrossRef]
- Zhou, G.S. Study on Resources Chemistry of Ginkgo biloba Seeds. Master’s Thesis, Nanjing University of Chinese Medicine, Nanjing, China, 2013. [Google Scholar]
- Tomova, T.; Doncheva, N.; Mihaylova, A.; Kostadinov, I.; Peychev, L.; Argirova, M. An experimental study on phytochemical composition and memory enhancing effect of Ginkgo biloba seed extract. Folia Med. 2021, 63, 203–212. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, Q.; Wang, J.; Sun, L.; Ba, B.; Shen, D. Mechanism of Astragalus membranaceus (Huangqi, HQ) for treatment of heart failure based on network pharmacology and molecular docking. J. Cell. Mol. Med. 2024, 28, e18331. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, J.; Shao, N.; Gao, Y.; Li, B.; Liang, Y.; Yang, Y.; Li, J. Mechanistic Investigation of Astragalus Root in the Management of T2DM-NAFLD Comorbidity: An Integrated Network Pharmacology, Molecular Docking, Molecular Dynamics Simulation, and In Vitro Study. Pharmaceuticals 2026, 19, 289. [Google Scholar] [CrossRef] [Scilit]
- Ma, C.; Wu, H.; Yang, G.; Xiang, J.; Feng, K.; Zhang, J.; Hua, Y.; Kang, L.; Fan, G.; Yang, S. Calycosin ameliorates atherosclerosis by enhancing autophagy via regulating the interaction between KLF2 and MLKL in apolipoprotein E gene-deleted mice. Br. J. Pharmacol. 2022, 179, 252–269. [Google Scholar] [CrossRef] [Scilit]
- Li, C.; He, Y.; Yang, Y.; Gou, Y.; Li, S.; Wang, R.; Zeng, S.; Zhao, X. Antioxidant and Inflammatory Effects of Nelumbo nucifera Gaertn. Leaves. Oxidaxive Med. Cell. Longev. 2021, 2021, 8375961. [Google Scholar] [CrossRef] [Scilit]
- Moore, G.; Brooks, P.; Pappalardo, L.; Boufridi, A. Phenolic profiles of Australian monofloral Eucalyptus, Corymbia, Macadamia and Lophostemon honeys via HPLC-DAD analysis. Food Chem. 2025, 462, 140900. [Google Scholar] [CrossRef] [Scilit]
- Gośliński, M.; Nowak, D.; Szwengiel, A. Multidimensional Comparative Analysis of Bioactive Phenolic Compounds of Honeys of Various Origin. Antioxidants 2021, 10, 530. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, J.; Tang, W.; Tang, W.; Gao, T.; Yuan, M.; Wu, Y.; Wang, G. Research progress on the types, functions, biosynthesis, and metabolic regulation of ginkgo terpenoids. Plant Physiol. Biochem. 2024, 212, 108754. [Google Scholar] [CrossRef] [Scilit]
- Forman, V.; Luo, D.; Geu-Flores, F.; Lemcke, R.; Nelson, D.R.; Kampranis, S.C.; Staerk, D.; Møller, B.L.; Pateraki, I. A gene cluster in Ginkgo biloba encodes unique multifunctional cytochrome P450s that initiate ginkgolide biosynthesis. Nat. Commun. 2022, 13, 5143. [Google Scholar] [CrossRef] [Scilit]
- Rather, L.J.; Mir, S.S.; Ganie, S.A.; Assiri, M.A.; Li, Q. Ginkgo biloba: The Traditional Use, Phytochemistry, Pharmacology, and Therapeutic Applications. Am. J. Chin. Med. 2025, 53, 2403–2434. [Google Scholar] [CrossRef] [Scilit]
- Liu, X.W.; Yang, J.L.; Niu, W.; Jia, W.W.; Olaleye, O.E.; Wen, Q.; Duan, X.N.; Huang, Y.H.; Wang, F.Q.; Du, F.F.; et al. Human pharmacokinetics of ginkgo terpene lactones and impact of carboxylation in blood on their platelet-activating factor antagonistic activity. Acta Pharmacol. Sin. 2018, 39, 1935–1946. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, W.Z.; Wu, W.Y.; Huang, H.; Wu, Y.Y.; Yin, Y.Y. Protective effect of bilobalide on learning and memory impairment in rats with vascular dementia. Mol. Med. Rep. 2013, 8, 935–941. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Salehi, B.; Carneiro, J.N.P.; Rocha, J.E.; Coutinho, H.D.M.; Morais Braga, M.F.B.; Sharifi-Rad, J.; Semwal, P.; Painuli, S.; Moujir, L.M.; de Zarate Machado, V.; et al. Astragalus species: Insights on its chemical composition toward pharmacological applications. Phytother. Res. 2021, 35, 2445–2476. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, S.; Hu, X.; Liu, F.; Hu, W. Bioactive components and clinical potential of Astragalus species. Front. Pharmacol. 2025, 16, 1585697. [Google Scholar] [CrossRef] [Scilit]
- Yang, C.; Pan, Q.; Ji, K.; Tian, Z.; Zhou, H.; Li, S.; Luo, C.; Li, J. Review on the protective mechanism of astragaloside IV against cardiovascular diseases. Front. Pharmacol. 2023, 14, 1187910. [Google Scholar] [CrossRef] [Scilit]
- Lin, X.P.; Cui, H.J.; Yang, A.L.; Luo, J.K.; Tang, T. Astragaloside IV Improves Vasodilatation Function by Regulating the PI3K/Akt/eNOS Signaling Pathway in Rat Aorta Endothelial Cells. J. Vasc. Res. 2018, 55, 169–176. [Google Scholar] [CrossRef] [Scilit]
- Meng, P.; Yang, R.; Jiang, F.; Guo, J.; Lu, X.; Yang, T.; He, Q. Molecular Mechanism of Astragaloside IV in Improving Endothelial Dysfunction of Cardiovascular Diseases Mediated by Oxidative Stress. Oxidaxive Med. Cell. Longev. 2021, 2021, 1481236. [Google Scholar] [CrossRef] [Scilit]
- Yao, J.; Liu, J.; He, Y.; Liu, L.; Xu, Z.; Lin, X.; Liu, N.; Kai, G. Systems pharmacology reveals the mechanism of Astragaloside IV in improving immune activity on cyclophosphamide-induced immunosuppressed mice. J. Ethnopharmacol. 2023, 313, 116533. [Google Scholar] [CrossRef] [Scilit]
- Pozzobon, R.G.; Rutckeviski, R.; de Lima, L.S.; Oliveira, C.S.; Smiderle, F.R. Anti-Inflammatory Potential of Ganoderma lucidum Triterpenes: A Systematic Review and Meta-Analysis of Preclinical Evidence. Pharmaceuticals 2026, 19, 188. [Google Scholar] [CrossRef] [Scilit]
- Hu, Z.; Du, R.; Xiu, L.; Bian, Z.; Ma, C.; Sato, N.; Hattori, M.; Zhang, H.; Liang, Y.; Yu, S.; et al. Protective effect of triterpenes of Ganoderma lucidum on lipopolysaccharide-induced inflammatory responses and acute liver injury. Cytokine 2020, 127, 154917. [Google Scholar] [CrossRef] [Scilit]
- Kim, H.; Ramirez, C.N.; Su, Z.Y.; Kong, A.N. Epigenetic modifications of triterpenoid ursolic acid in activating Nrf2 and blocking cellular transformation of mouse epidermal cells. J. Nutr. Biochem. 2016, 33, 54–62. [Google Scholar] [CrossRef] [Scilit]
- Krajka-Kuźniak, V.; Paluszczak, J.; Oszmiański, J.; Baer-Dubowska, W. Hawthorn (Crataegus oxyacantha L.) bark extract regulates antioxidant response element (ARE)-mediated enzyme expression via Nrf2 pathway activation in normal hepatocyte cell line. Phytother. Res. 2014, 28, 593–602. [Google Scholar] [CrossRef] [Scilit]
- Reisman, S.A.; Aleksunes, L.M.; Klaassen, C.D. Oleanolic acid activates Nrf2 and protects from acetaminophen hepatotoxicity via Nrf2-dependent and Nrf2-independent processes. Biochem. Pharmacol. 2009, 77, 1273–1282. [Google Scholar] [CrossRef] [Scilit]
- Xu, L.; Xiao, S.; Sun, R.; Li, Z.; Feng, Z.; Cheng, J.; Yang, L.; Ma, C.; Fan, H.; Chai, Z. Assessment of the structural characterization and anti-inflammatory activities of various parts of Astragalus (root, stem, leaf, flower) from a polysaccharide perspective. Int. J. Biol. Macromol. 2026, 339, 149904. [Google Scholar] [CrossRef] [Scilit]
- Li, C.X.; Liu, Y.; Zhang, Y.Z.; Li, J.C.; Lai, J. Astragalus polysaccharide: A review of its immunomodulatory effect. Arch. Pharm. Res. 2022, 45, 367–389. [Google Scholar] [CrossRef] [Scilit]
- Sha, W.; Zhao, B.; Wei, H.; Yang, Y.; Yin, H.; Gao, J.; Zhao, W.; Kong, W.; Ge, G.; Lei, T. Astragalus polysaccharide ameliorates vascular endothelial dysfunction by stimulating macrophage M2 polarization via potentiating Nrf2/HO-1 signaling pathway. Phytomedicine 2023, 112, 154667. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, G.; Jiang, N.; Zheng, J.; Hu, H.; Yang, H.; Lin, A.; Hu, B.; Liu, H. Structural characterization and anti-inflammatory activity of polysaccharides from Astragalus membranaceus. Int. J. Biol. Macromol. 2023, 241, 124386. [Google Scholar] [CrossRef] [Scilit]
- Yang, M.; Qin, X.; Liu, X. A review of polysaccharides from Ganoderma lucidum: Preparation methods, structural characteristics, bioactivities, structure-activity relationships and potential applications. Int. J. Biol. Macromol. 2025, 303, 140645. [Google Scholar] [CrossRef] [Scilit]
- Ren, L.; Zhang, J.; Zhang, T. Immunomodulatory activities of polysaccharides from Ganoderma on immune effector cells. Food Chem. 2021, 340, 127933. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, J.; Gu, F.; Cai, C.; Hu, M.; Fan, L.; Hao, J.; Yu, G. Purification, structural characterization, and immunomodulatory activity of the polysaccharides from Ganoderma lucidum. Int. J. Biol. Macromol. 2020, 143, 806–813. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Y.; Zuo, Y.; Weng, J.; Peng, X. Health benefits of Ganoderma lucidum polysaccharides: A review of potential cardiovascular protective effects. Int. J. Biol. Macromol. 2025, 330, 148001. [Google Scholar] [CrossRef] [Scilit]
- Li, L.F.; Liu, H.B.; Zhang, Q.W.; Li, Z.P.; Wong, T.L.; Fung, H.Y.; Zhang, J.X.; Bai, S.P.; Lu, A.P.; Han, Q.B. Comprehensive comparison of polysaccharides from Ganoderma lucidum and G. sinense: Chemical, antitumor, immunomodulating and gut-microbiota modulatory properties. Sci. Rep. 2018, 8, 6172. [Google Scholar] [CrossRef] [Scilit]
- Wang, B.; Yang, J.; Tao, L.; Zhou, X.; Ding, X. Structural-activity relationship of Lycium barbarum polysaccharides in immunomodulation: Integrating molecular insights with target identification for therapeutic development. Front. Immunol. 2026, 17, 1730418. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Y.; Yang, B.; Zhang, X.; Shen, X.; Ma, Y.; Jing, L. Lycium barbarum polysaccharide antagonizes cardiomyocyte apoptosis by inhibiting the upregulation of GRK2 induced by I/R injury, and salvage mitochondrial fission/fusion imbalance and AKT/eNOS signaling. Cell Signal. 2022, 92, 110252. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ke, Y.; Lin, L.; Zhao, M. Rhamnogalacturonan I-Enriched Pectin, Flavonoids, and Alkaloids from Lotus Leaf Infusion in Regulating Glycolipid Absorption and Metabolism: Isolation, In Vitro Bioactivity Verification, and Structural Characterization. J. Agric. Food Chem. 2023, 71, 8969–8980. [Google Scholar] [CrossRef] [Scilit]
- Gunness, P.; Gidley, M.J. Mechanisms underlying the cholesterol-lowering properties of soluble dietary fibre polysaccharides. Food Funct. 2010, 1, 149–155. [Google Scholar] [CrossRef] [Scilit]
- Falk, J.D.; Nagyvary, J.J. Exploratory studies of lipid-pectin interactions. J. Nutr. 1982, 112, 182–188. [Google Scholar] [CrossRef] [Scilit]
- Kern, F., Jr.; Birkner, H.J.; Ostrower, V.S. Binding of bile acids by dietary fiber. Am. J. Clin. Nutr. 1978, 31, S175–S179. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Story, J.A.; Kritchevsky, D. Comparison of the binding of various bile acids and bile salts in vitro by several types of fiber. J. Nutr. 1976, 106, 1292–1294. [Google Scholar] [CrossRef] [Scilit]
- Chen, M.M.; Dong, S.; Wang, K.W.; Zhou, T. Physicochemical and functional properties of octenyl succinic anhydride-modified polysaccharides from fermented lotus leaves. Int. J. Biol. Macromol. 2026, 344, 150509. [Google Scholar] [CrossRef] [Scilit]
- Hong, Q.; Ma, Z.C.; Huang, H.; Wang, Y.G.; Tan, H.L.; Xiao, C.R.; Liang, Q.D.; Zhang, H.T.; Gao, Y. Antithrombotic activities of ferulic acid via intracellular cyclic nucleotide signaling. Eur. J. Pharmacol. 2016, 777, 1–8. [Google Scholar] [CrossRef] [Scilit]
- Li, W.J.; Cai, Y.F.; Ouyang, Y.; Li, X.Y.; Shi, X.L.; Cao, S.X.; Huang, Y.; Wu, H.W.; Yang, H.J. Quality evaluation of Angelica Sinensis Radix dispensing granules by integrating microvascular activity and chemical analysis. J. Ethnopharmacol. 2024, 319, 117236. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- An, W.; Tian, Q.; Guo, P.; Chen, M.; Zhang, T.; Yang, P.; Zhang, S. Danggui Buxue Decoction and its components dilate coronary artery through activating the inward rectification K+ channels pathway. J. Ethnopharmacol. 2025, 338, 119064. [Google Scholar] [CrossRef] [Scilit]
- Zhang, K.; Shen, X.; Yang, L.; Chen, Q.; Wang, N.; Li, Y.; Song, P.; Jiang, M.; Bai, G.; Yang, P.; et al. Exploring the Q-markers of Angelica sinensis (Oliv.) Diels of anti-platelet aggregation activity based on spectrum–effect relationships. Biomed. Chromatogr. 2022, 36, e5422. [Google Scholar] [CrossRef] [Scilit]
- Singh, A.K.; Singla, R.K.; Pandey, A.K. Chlorogenic Acid: A Dietary Phenolic Acid with Promising Pharmacotherapeutic Potential. Curr. Med. Chem. 2023, 30, 3905–3926. [Google Scholar] [CrossRef] [Scilit]
- Vardhini, N.M.; Punia, J.; Jat, S.; Pawar, S.D.; Devi, N.; Radhakrishnanand, P.; Murty, U.S.; Saini, A.; Sethi, K.K.; Kumar, P. Purification and characterization of pure curcumin, desmethoxycurcumin, and bisdemethoxycurcumin from North-East India Lakadong turmeric (Curcuma longa). J. Chromatogr. A 2023, 1708, 464358. [Google Scholar] [CrossRef] [Scilit]
- Praveen, A.; Prasad, D.; Mishra, S.; Nagarajan, S.; Chaudhari, S.R. Facile NMR approach for profiling curcuminoids present in turmeric. Food Chem. 2021, 341, 128646. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Younis, H.M.; Mohamed, A.A. A Review on Curcumin: Pharmacological Promises and Biomedical Activities. Arch. Pharm. 2025, 358, e70129. [Google Scholar] [CrossRef] [Scilit]
- El-Saadony, M.T.; Saad, A.M.; Mohammed, D.M.; Alkafaas, S.S.; Ghosh, S.; Negm, S.H.; Salem, H.M.; Fahmy, M.A.; Mosa, W.F.A.; Ibrahim, E.H.; et al. Curcumin, an active component of turmeric: Biological activities, nutritional aspects, immunological, bioavailability, and human health benefits—A comprehensive review. Front. Immunol. 2025, 16, 1603018. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pan-On, S.; Dilokthornsakul, P.; Tiyaboonchai, W. Trends in advanced oral drug delivery system for curcumin: A systematic review. J. Control. Release 2022, 348, 335–345. [Google Scholar] [CrossRef] [Scilit]
- Saavedra, D.I.; Carter, D.T.; Dawson, J.T.; Shah, S.A.; Stevens, N.; Poudel, A.; Satyal, P.; Bascoul, C. Turmeric (Curcuma longa) rhizome essential oil: Analytical profile of authenticated and commercial samples, safety and pharmacology review. Pharm. Biol. 2026, 64, 379–397. [Google Scholar] [CrossRef] [Scilit]
- Gao, Y.; Lu, Y.; Zhang, N.; Udenigwe, C.C.; Zhang, Y.; Fu, Y. Preparation, pungency and bioactivity of gingerols from ginger (Zingiber officinale Roscoe): A review. Crit. Rev. Food Sci. Nutr. 2024, 64, 2708–2733. [Google Scholar] [CrossRef] [Scilit]
- Garza-Cadena, C.; Ortega-Rivera, D.M.; Machorro-García, G.; Gonzalez-Zermeño, E.M.; Homma-Dueñas, D.; Plata-Gryl, M.; Castro-Muñoz, R. A comprehensive review on Ginger (Zingiber officinale) as a potential source of nutraceuticals for food formulations: Towards the polishing of gingerol and other present biomolecules. Food Chem. 2023, 413, 135629. [Google Scholar] [CrossRef] [Scilit]
- Krüger, S.; Bergin, A.; Morlock, G.E. Effect-directed analysis of ginger (Zingiber officinale) and its food products, and quantification of bioactive compounds via high-performance thin-layer chromatography and mass spectrometry. Food Chem. 2018, 243, 258–268. [Google Scholar] [CrossRef] [Scilit]
- He, X.; Shang, Y.; Liao, X.; Liu, G.; Yang, Q.; Liu, J.; Xu, X.; Liu, X. 6-Gingerol ameliorates endothelial injury in hyperlipidemia mice via Nrf2 activation and inflammation modulation. Food Funct. 2026, 17, 1007–1017. [Google Scholar] [CrossRef] [Scilit]
- Ahmed, S.H.H.; Gonda, T.; Agbadua, O.G.; Girst, G.; Berkecz, R.; Kúsz, N.; Tsai, M.C.; Wu, C.C.; Balogh, G.T.; Hunyadi, A. Preparation and Evaluation of 6-Gingerol Derivatives as Novel Antioxidants and Antiplatelet Agents. Antioxidants 2023, 12, 744. [Google Scholar] [CrossRef] [Scilit]
- Sang, S.; Snook, H.D.; Tareq, F.S.; Fasina, Y. Precision Research on Ginger: The Type of Ginger Matters. J. Agric. Food Chem. 2020, 68, 8517–8523. [Google Scholar] [CrossRef] [Scilit]
- Bischoff-Kont, I.; Fürst, R. Benefits of Ginger and Its Constituent 6-Shogaol in Inhibiting Inflammatory Processes. Pharmaceuticals 2021, 14, 571. [Google Scholar] [CrossRef] [Scilit]
- Du, Y.T.; Zheng, Y.L.; Ji, Y.; Dai, F.; Hu, Y.J.; Zhou, B. Applying an Electrophilicity-Based Strategy to Develop a Novel Nrf2 Activator Inspired from Dietary [6]-Shogaol. J. Agric. Food Chem. 2018, 66, 7983–7994. [Google Scholar] [CrossRef] [Scilit]
- Bratosin, E.D.; Tit, D.M.; Purza, A.L.; Pasca, M.B.; Bungau, G.S.; Marin, R.C.; Radu, A.F.; Gitea, D. Exploratory Analysis of Phenolic Profiles and Antioxidant Capacity in Selected Romanian Monofloral Honeys: Influence of Botanical Origin and Acquisition Source. Antioxidants 2025, 14, 1248. [Google Scholar] [CrossRef] [Scilit]
- Combarros-Fuertes, P.; Estevinho, L.M.; Dias, L.G.; Castro, J.M.; Tomás-Barberán, F.A.; Tornadijo, M.E.; Fresno-Baro, J.M. Bioactive Components and Antioxidant and Antibacterial Activities of Different Varieties of Honey: A Screening Prior to Clinical Application. J. Agric. Food Chem. 2019, 67, 688–698. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Li, W.; Wu, Y.; Wu, H.; Cai, X. Integrating network pharmacology and animal experimental validation to investigate the mechanism of lotus leaf in obesity. Int. Immunopharmacol. 2025, 145, 113719. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Inchan, A.; Bualeong, T.; Kaewkong, W.; Nuengchamnong, N.; Apaikawee, P.; Sa-Nguanpong, P.; Sumsakul, W.; Charoenphon, N.; Chatturong, U.; Deetud, W.; et al. Antihypertensive Effects of Lotus Seed (Nelumbo nucifera Gaertn.) Extract via eNOS Upregulation and Oxidative Stress Reduction in L-NAME-Induced Hypertensive Rats. Pharm. 2025, 18, 1156. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wicha, P.; Onsa-Ard, A.; Chaichompoo, W.; Suksamrarn, A.; Tocharus, C. Vasorelaxant and Antihypertensive Effects of Neferine in Rats: An In Vitro and In Vivo Study. Planta Med. 2020, 86, 496–504. [Google Scholar] [CrossRef] [Scilit]
- Ma, R.H.; Zhang, X.X.; Ni, Z.J.; Thakur, K.; Wang, W.; Yan, Y.M.; Cao, Y.L.; Zhang, J.G.; Rengasamy, K.R.R.; Wei, Z.J. Lycium barbarum (Goji) as functional food: A review of its nutrition, phytochemical structure, biological features, and food industry prospects. Crit. Rev. Food Sci. Nutr. 2023, 63, 10621–10635. [Google Scholar] [CrossRef] [Scilit]
- Zhu, X.; Cheang, I.; Tang, Y.; Shi, M.; Zhu, Q.; Gao, R.; Liao, S.; Yao, W.; Zhou, Y.; Zhang, H.; et al. Associations of Serum Carotenoids with Risk of All-Cause and Cardiovascular Mortality in Hypertensive Adults. J. Am. Heart Assoc. 2023, 12, e027568. [Google Scholar] [CrossRef] [Scilit]
- Parichatikanond, W.; Duangrat, R.; Nuamnaichati, N.; Mangmool, S. Role of A(1) adenosine receptor in cardiovascular diseases: Bridging molecular mechanisms with therapeutic opportunities. Exp. Mol. Pathol. 2025, 141, 104952. [Google Scholar] [CrossRef] [Scilit]
- Borea, P.A.; Gessi, S.; Merighi, S.; Varani, K. Adenosine as a Multi-Signalling Guardian Angel in Human Diseases: When, Where and How Does it Exert its Protective Effects? Trends Pharmacol. Sci. 2016, 37, 419–434. [Google Scholar] [CrossRef] [Scilit]
- Girma, A.; Seo, W.; She, R.C. Antibacterial activity of varying UMF-graded Manuka honeys. PLoS ONE 2019, 14, e0224495. [Google Scholar] [CrossRef] [Scilit]
- Leng, B.; Tang, F.; Lu, M.; Zhang, Z.; Wang, H.; Zhang, Y. Astragaloside IV improves vascular endothelial dysfunction by inhibiting the TLR4/NF-κB signaling pathway. Life Sci. 2018, 209, 111–121. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liperoti, R.; Vetrano, D.L.; Bernabei, R.; Onder, G. Herbal Medications in Cardiovascular Medicine. J. Am. Coll. Cardiol. 2017, 69, 1188–1199. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Choi, E.S.; Yoon, J.J.; Han, B.H.; Jeong, D.H.; Lee, Y.J.; Kang, D.G.; Lee, H.S. Ligustilide attenuates vascular inflammation and activates Nrf2/HO-1 induction and, NO synthesis in HUVECs. Phytomedicine 2018, 38, 12–23. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Moore, K.J.; Koplev, S.; Fisher, E.A.; Tabas, I.; Björkegren, J.L.M.; Doran, A.C.; Kovacic, J.C. Macrophage Trafficking, Inflammatory Resolution, and Genomics in Atherosclerosis: JACC Macrophage in CVD Series (Part 2). J. Am. Coll. Cardiol. 2018, 72, 2181–2197. [Google Scholar] [CrossRef] [Scilit]
- Bischoff-Kont, I.; Primke, T.; Niebergall, L.S.; Zech, T.; Fürst, R. Ginger Constituent 6-Shogaol Inhibits Inflammation- and Angiogenesis-Related Cell Functions in Primary Human Endothelial Cells. Front. Pharmacol. 2022, 13, 844767. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, S.; Chen, B.; Wu, W.; Bao, L.; Qi, R. Ginkgolide B reduces inflammatory protein expression in oxidized low-density lipoprotein-stimulated human vascular endothelial cells. J. Cardiovasc. Pharmacol. 2011, 57, 721–727. [Google Scholar] [CrossRef] [Scilit]
- Feng, Z.; Yang, X.; Zhang, L.; Ansari, I.A.; Khan, M.S.; Han, S.; Feng, Y. Ginkgolide B ameliorates oxidized low-density lipoprotein-induced endothelial dysfunction via modulating Lectin-like ox-LDL-receptor-1 and NADPH oxidase 4 expression and inflammatory cascades. Phytother. Res. 2018, 32, 2417–2427. [Google Scholar] [CrossRef] [Scilit]
- Hu, H.; Weng, J.; Cui, C.; Tang, F.; Yu, M.; Zhou, Y.; Shao, F.; Zhu, Y. The Hypolipidemic Effect of Hawthorn Leaf Flavonoids through Modulating Lipid Metabolism and Gut Microbiota in Hyperlipidemic Rats. Evid. Based Complement. Altern. Med. 2022, 2022, 3033311. [Google Scholar] [CrossRef] [Scilit]
- Chen, B.; Tian, J.; Zhang, J.; Wang, K.; Liu, L.; Yang, B.; Bao, L.; Liu, H. Triterpenes and meroterpenes from Ganoderma lucidum with inhibitory activity against HMGs reductase, aldose reductase and α-glucosidase. Fitoterapia 2017, 120, 6–16. [Google Scholar] [CrossRef] [Scilit]
- Zhu, J.; Jin, J.; Ding, J.; Li, S.; Cen, P.; Wang, K.; Wang, H.; Xia, J. Ganoderic Acid A improves high fat diet-induced obesity, lipid accumulation and insulin sensitivity through regulating SREBP pathway. Chem. Biol. Interact. 2018, 290, 77–87. [Google Scholar] [CrossRef] [Scilit]
- Yu, X.H.; Tang, C.K. ABCA1, ABCG1, and Cholesterol Homeostasis. Adv. Exp. Med. Biol. 2022, 1377, 95–107. [Google Scholar] [CrossRef] [Scilit]
- Dergunov, A.D.; Baserova, V.B. Different Pathways of Cellular Cholesterol Efflux. Cell Biochem. Biophys. 2022, 80, 471–481. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, S.M.; Moon, J.; Cho, Y.; Chung, J.H.; Shin, M.J. Quercetin up-regulates expressions of peroxisome proliferator-activated receptor γ, liver X receptor α, and ATP binding cassette transporter A1 genes and increases cholesterol efflux in human macrophage cell line. Nutr. Res. 2013, 33, 136–143. [Google Scholar] [CrossRef] [Scilit]
- Dong, P.; Pan, L.; Zhang, X.; Zhang, W.; Wang, X.; Jiang, M.; Chen, Y.; Duan, Y.; Wu, H.; Xu, Y.; et al. Hawthorn (Crataegus pinnatifida Bunge) leave flavonoids attenuate atherosclerosis development in apoE knock-out mice. J. Ethnopharmacol. 2017, 198, 479–488. [Google Scholar] [CrossRef] [Scilit]
- Wang, W.; Sun, R.; Zhang, J.; Jia, L.; Dong, Y. Study on the Mechanism of Ganoderma lucidum Polysaccharides for Ameliorating Dyslipidemia via Regulating Gut Microbiota and Fecal Metabolites. Biomolecules 2026, 16, 153. [Google Scholar] [CrossRef] [Scilit]
- Zhang, S.; Zou, J.; Li, P.; Zheng, X.; Feng, D. Curcumin Protects against Atherosclerosis in Apolipoprotein E-Knockout Mice by Inhibiting Toll-like Receptor 4 Expression. J. Agric. Food Chem. 2018, 66, 449–456. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nievergelt, A.; Marazzi, J.; Schoop, R.; Altmann, K.H.; Gertsch, J. Ginger phenylpropanoids inhibit IL-1beta and prostanoid secretion and disrupt arachidonate-phospholipid remodeling by targeting phospholipases A2. J. Immunol. 2011, 187, 4140–4150. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, X.; Zhao, G.; Yan, Y.; Bao, L.; Chen, B.; Qi, R. Ginkgolide B reduces atherogenesis and vascular inflammation in ApoE−/− mice. PLoS ONE 2012, 7, e36237. [Google Scholar] [CrossRef] [Scilit]
- Yin, H.; Guo, Q.; Li, X.; Tang, T.; Li, C.; Wang, H.; Sun, Y.; Feng, Q.; Ma, C.; Gao, C.; et al. Curcumin Suppresses IL-1β Secretion and Prevents Inflammation through Inhibition of the NLRP3 Inflammasome. J. Immunol. 2018, 200, 2835–2846. [Google Scholar] [CrossRef] [Scilit]
- Wu, J.; He, S.; Song, Z.; Chen, S.; Lin, X.; Sun, H.; Zhou, P.; Peng, Q.; Du, S.; Zheng, S.; et al. Macrophage polarization states in atherosclerosis. Front. Immunol. 2023, 14, 1185587. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Liu, S.; Kong, F.; Shu, L.; Li, Y.; Wang, D.; Li, L. Acidic polysaccharide from Ganoderma tsugae: Structural characterization and antiatherosclerotic related to macrophage polarization. Food Res. Int. 2025, 203, 115913. [Google Scholar] [CrossRef] [Scilit]
- Quan, Y.Z.; Ma, A.; Ren, C.Q.; An, Y.P.; Qiao, P.S.; Gao, C.; Zhang, Y.K.; Li, X.W.; Lin, S.M.; Li, N.N.; et al. Ganoderic acids alleviate atherosclerosis by inhibiting macrophage M1 polarization via TLR4/MyD88/NF-κB signaling pathway. Atherosclerosis 2024, 391, 117478. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, L.; Yang, J.; Liu, H.; Rang, Y.; Xu, L.; Wang, X.; Li, Y.; Liu, C. Lycium barbarum polysaccharides attenuate oxidative stress and mitochondrial toxicity induced by mixed plasticizers in HepG2 cells through activation of Nrf2. Life Sci. 2024, 336, 122346. [Google Scholar] [CrossRef] [Scilit]
- Yang, Y.; Yu, L.; Zhu, T.; Xu, S.; He, J.; Mao, N.; Liu, Z.; Wang, D. Neuroprotective effects of Lycium barbarum polysaccharide on light-induced oxidative stress and mitochondrial damage via the Nrf2/HO-1 pathway in mouse hippocampal neurons. Int. J. Biol. Macromol. 2023, 251, 126315. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Wang, F.; Xu, H.; Wang, H.; Lu, M.; Cheng, L. Ginkgolide B attenuates hyperlipidemia by restoring sphingolipid homeostasis and activating PPARα and Nrf2 pathways. Sci. Rep. 2025, 15, 28774. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, L.; Wang, X.; Meng, C.; Li, T.; Wang, Q.; Zhang, M.; Wu, M. Exploring the role of curcumin in anti-atherosclerosis: Mechanisms and pathways of action. Phytomedicine 2026, 152, 157809. [Google Scholar] [CrossRef] [Scilit]
- Wu, S.; Liao, X.; Zhu, Z.; Huang, R.; Chen, M.; Huang, A.; Zhang, J.; Wu, Q.; Wang, J.; Ding, Y. Antioxidant and anti-inflammation effects of dietary phytochemicals: The Nrf2/NF-κB signalling pathway and upstream factors of Nrf2. Phytochemistry 2022, 204, 113429. [Google Scholar] [CrossRef] [Scilit]
- Battino, M.; Giampieri, F.; Cianciosi, D.; Ansary, J.; Chen, X.; Zhang, D.; Gil, E.; Forbes-Hernández, T. The roles of strawberry and honey phytochemicals on human health: A possible clue on the molecular mechanisms involved in the prevention of oxidative stress and inflammation. Phytomedicine 2021, 86, 153170. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, J.; Han, B.; Zhao, S.; Zhong, Y.; Han, W.; Gao, J.; Wang, S. Bioactive characterization of multifloral honeys from Apis cerana cerana, Apis dorsata, and Lepidotrigona flavibasis. Food Res. Int. 2022, 161, 111808. [Google Scholar] [CrossRef] [Scilit]
- Ma, L.; Liu, X.; Zhao, Y.; Chen, B.; Li, X.; Qi, R. Ginkgolide B reduces LOX-1 expression by inhibiting Akt phosphorylation and increasing Sirt1 expression in oxidized LDL-stimulated human umbilical vein endothelial cells. PLoS ONE 2013, 8, e74769. [Google Scholar] [CrossRef] [Scilit]
- Bai, X.; Wang, S.; Shu, L.; Cao, Q.; Hu, H.; Zhu, Y.; Chen, C. Hawthorn leaf flavonoids alleviate the deterioration of atherosclerosis by inhibiting SCAP-SREBP2-LDLR pathway through sPLA2-IIA signaling in macrophages in mice. J. Ethnopharmacol. 2024, 327, 118006. [Google Scholar] [CrossRef] [Scilit]
- Kremastiotis, G.; Handa, I.; Jackson, C.; George, S.; Johnson, J. Disparate effects of MMP and TIMP modulation on coronary atherosclerosis and associated myocardial fibrosis. Sci. Rep. 2021, 11, 23081. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Lai, G.; Guo, Y.; Tang, X.; Shuai, O.; Xie, Y.; Wu, Q.; Chen, D.; Yuan, X. Protective effect of Ganoderma lucidum spore extract in trimethylamine-N-oxide-induced cardiac dysfunction in rats. J. Food Sci. 2021, 86, 546–562. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sang, T.; Guo, C.; Guo, D.; Wu, J.; Wang, Y.; Wang, Y.; Chen, J.; Chen, C.; Wu, K.; Na, K.; et al. Suppression of obesity and inflammation by polysaccharide from sporoderm-broken spore of Ganoderma lucidum via gut microbiota regulation. Carbohydr. Polym. 2021, 256, 117594. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jiang, T.; Zhu, R.; Guo, X.; Li, J.; Zhu, X.; Bao, R.; Chen, J. Comprehensive evaluation of Ganoderma lucidum extracts: Digestion kinetics, gut microbiota modulation, and immunoregulatory mechanisms. Food Res. Int. 2026, 230, 118664. [Google Scholar] [CrossRef] [Scilit]
- Wang, Z.; Ren, X.; Peng, Z.; Zeng, M.; Wang, Z.; Chen, Q.; Chen, J.; Dai, X.; Christian, M.; Qie, X.; et al. Flavonoid-rich extracts of Nelumbo nucifera leaves alleviate obesity in HFD-fed mice via microbiota-dependent modulation of brown fat thermogenesis. J. Ethnopharmacol. 2026, 354, 120513. [Google Scholar] [CrossRef] [Scilit]
- Shi, D.; Xu, X.; Wang, J.; Bu, T.; Sun, P.; Yang, K.; Cai, M. Synergistic anti-inflammatory effects of Ganoderma lucidum polysaccharide and ganoderic acid A on LPS-induced RAW264.7 cells by inhibition of TLR4/NF-κB activation. Int. J. Biol. Macromol. 2025, 309, 143074. [Google Scholar] [CrossRef] [Scilit]
- Li, Y.; Tang, J.; Gao, H.; Xu, Y.; Han, Y.; Shang, H.; Lu, Y.; Qin, C. Ganoderma lucidum triterpenoids and polysaccharides attenuate atherosclerotic plaque in high-fat diet rabbits. Nutr. Metab. Cardiovasc. Dis. 2021, 31, 1929–1938. [Google Scholar] [CrossRef] [Scilit]
- Caruso, L.; Nadur, N.F.; da Fonseca, M.B.; Peixoto Ferreira, L.A.; Lacerda, R.B.; Graebin, C.S.; Kümmerle, A.E. The Design of Multi-target Drugs to Treat Cardiovascular Diseases: Two (or more) Birds on One Stone. Curr. Top. Med. Chem. 2022, 22, 366–394. [Google Scholar] [CrossRef] [Scilit]
- Peters, J.U. Polypharmacology—Foe or friend? J. Med. Chem. 2013, 56, 8955–8971. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, S.; Yang, H.; Zhang, Y. Yao-Shan of traditional Chinese medicine: An old story for metabolic health. Front. Pharmacol. 2023, 14, 1194026. [Google Scholar] [CrossRef] [Scilit]
- Li, Y.; Xu, Z.; Du, P.; Gao, J.; Wang, S.; Pang, X.; Ren, C.; Liu, Y.; Zhang, C. Methodological challenges in pilot trials of herbal medicine: Barriers to evidence-based practice. J. Clin. Epidemiol. 2025, 182, 111754. [Google Scholar] [CrossRef] [Scilit]
- Unhapipatpong, C.; Julanon, N.; Shantavasinkul, P.C.; Polruang, N.; Numthavaj, P.; Thakkinstian, A. An Umbrella Review of Systematic Reviews and Meta-analyses of Randomized Controlled Trials Investigating the Effect of Curcumin Supplementation on Lipid Profiles. Nutr. Rev. 2025, 83, 1520–1536. [Google Scholar] [CrossRef] [Scilit]
- Blumenthal, R.S.; Morris, P.B.; Gaudino, M.; Johnson, H.M.; Anderson, T.S.; Bittner, V.A.; Blankstein, R.; Brewer, L.C.; Cho, L.; Ferranti, S.D.d.; et al. 2026 ACC/AHA/AACVPR/ABC/ACPM/ADA/AGS/APhA/ASPC/NLA/PCNA Guideline on the Management of Dyslipidemia. JACC 2026, 87, 2624–2757. [Google Scholar] [CrossRef] [Scilit]
- Zeng, X.; Zhao, W.; Wang, S.; Xiong, H.; Wu, J.; Ren, J.L. barbarum (Lycium barbarum L.) supplementation for lipid profiles in adults: A systematic review and meta-analysis of RCTs. Medicine 2023, 102, e34952. [Google Scholar] [CrossRef] [Scilit]
- Toh, D.W.K.; Low, J.H.M.; Kim, J.E. Cardiovascular disease risk reduction with wolfberry consumption: A systematic review and meta-analysis of randomized controlled trials. Eur. J. Nutr. 2022, 61, 1177–1186. [Google Scholar] [CrossRef] [Scilit]
- Klupp, N.L.; Chang, D.; Hawke, F.; Kiat, H.; Cao, H.; Grant, S.J.; Bensoussan, A. Ganoderma lucidum mushroom for the treatment of cardiovascular risk factors. Cochrane Database Syst. Rev. 2015, 2015, CD007259. [Google Scholar] [CrossRef] [Scilit]
- Han, X.; Yu, T.; Chen, X.; Du, Z.; Yu, M.; Xiong, J. Effect of Astragalus membranaceus on left ventricular remodeling in HFrEF: A systematic review and meta-analysis. Front. Pharmacol. 2024, 15, 1345797. [Google Scholar] [CrossRef] [Scilit]
- Wei, H.; Xiao, Y.; Tong, Y.; Chen, Y.; Luo, X.; Wang, Y.; Jin, P.; Ma, C.; Fu, Z.; Guo, H.; et al. Therapeutic effect of angelica and its compound formulas for hypertension and the complications: Evidence mapping. Phytomedicine 2019, 59, 152767. [Google Scholar] [CrossRef] [Scilit]
- Ma, Z.; Wang, N.; He, H.; Tang, X. Pharmaceutical strategies of improving oral systemic bioavailability of curcumin for clinical application. J. Control. Release 2019, 316, 359–380. [Google Scholar] [CrossRef] [Scilit]
- Tan, O.J.; Loo, H.L.; Thiagarajah, G.; Palanisamy, U.D.; Sundralingam, U. Improving oral bioavailability of medicinal herbal compounds through lipid-based formulations—A Scoping Review. Phytomedicine 2021, 90, 153651. [Google Scholar] [CrossRef] [Scilit]
- Flory, S.; Sus, N.; Haas, K.; Jehle, S.; Kienhöfer, E.; Waehler, R.; Adler, G.; Venturelli, S.; Frank, J. Increasing Post-Digestive Solubility of Curcumin Is the Most Successful Strategy to Improve its Oral Bioavailability: A Randomized Cross-Over Trial in Healthy Adults and In Vitro Bioaccessibility Experiments. Mol. Nutr. Food Res. 2021, 65, e2100613. [Google Scholar] [CrossRef] [Scilit]
- Preciado Iñiga, G.; Martínez-Carrera, D.; Meneses, M.E.; Sánchez, M.; Argumedo, A.; Bonilla, M.; Castillo, I.; Petlacalco, B.; Morales, A.; Fernández, N.; et al. Characterisation and Hypolipidaemic Effects of Tlayudas, Widely Consumed Tortillas, Containing Ganoderma lucidum Extracts on an In Vivo Model of Hypercholesterolaemia. Int. J. Food Sci. 2025, 2025, 8096060. [Google Scholar] [CrossRef] [Scilit]
- Ahmed, A.; Tul-Noor, Z.; Lee, D.; Bajwah, S.; Ahmed, Z.; Zafar, S.; Syeda, M.; Jamil, F.; Qureshi, F.; Zia, F.; et al. Effect of honey on cardiometabolic risk factors: A systematic review and meta-analysis. Nutr. Rev. 2023, 81, 758–774. [Google Scholar] [CrossRef] [Scilit]
- Villaescusa, L.; Zaragozá, C.; Zaragozá, F.; Tamargo, J. Herbal medicines for the treatment of cardiovascular diseases: Benefits and risks—A narrative review. Int. J. Cardiol. 2023, 385, 44–52. [Google Scholar] [CrossRef] [Scilit]
- De Smet, P.A.G.M. Herbal Remedies. N. Engl. J. Med. 2002, 347, 2046–2056. [Google Scholar] [CrossRef] [Scilit]
- Chow, S.L.; Bozkurt, B.; Baker, W.L.; Bleske, B.E.; Breathett, K.; Fonarow, G.C.; Greenberg, B.; Khazanie, P.; Leclerc, J.; Morris, A.A.; et al. Complementary and Alternative Medicines in the Management of Heart Failure: A Scientific Statement From the American Heart Association. Circulation 2023, 147, e4–e30. [Google Scholar] [CrossRef] [Scilit]
- Boateng, I.D. A critical review of current technologies used to reduce ginkgotoxin, ginkgotoxin-5′-glucoside, ginkgolic acid, allergic glycoprotein, and cyanide in Ginkgo biloba L. seed. Food Chem. 2022, 382, 132408. [Google Scholar] [CrossRef] [Scilit]
- Azuma, F.; Nokura, K.; Kako, T.; Kobayashi, D.; Yoshimura, T.; Wada, K. An Adult Case of Generalized Convulsions Caused by the Ingestion of Ginkgo biloba Seeds with Alcohol. Intern. Med. 2020, 59, 1555–1558. [Google Scholar] [CrossRef] [Scilit]
- Kajiyama, Y.; Fujii, K.; Takeuchi, H.; Manabe, Y. Ginkgo seed poisoning. Pediatrics 2002, 109, 325–327. [Google Scholar] [CrossRef] [Scilit]
- Bone, K.M. Potential interaction of Ginkgo biloba leaf with antiplatelet or anticoagulant drugs: What is the evidence? Mol. Nutr. Food Res. 2008, 52, 764–771. [Google Scholar] [CrossRef] [Scilit]
- Kuller, L.H.; Ives, D.G.; Fitzpatrick, A.L.; Carlson, M.C.; Mercado, C.; Lopez, O.L.; Burke, G.L.; Furberg, C.D.; DeKosky, S.T. Does Ginkgo biloba reduce the risk of cardiovascular events? Circ. Cardiovasc. Qual. Outcomes 2010, 3, 41–47. [Google Scholar] [CrossRef] [Scilit]
- Crichton, M.; Davidson, A.R.; Innerarity, C.; Marx, W.; Lohning, A.; Isenring, E.; Marshall, S. Orally consumed ginger and human health: An umbrella review. Am. J. Clin. Nutr. 2022, 115, 1511–1527. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Burkina, V.; Zamaratskaia, G.; Rasmussen, M.K. Curcumin and quercetin modify warfarin-induced regulation of porcine CYP1A2 and CYP3A expression and activity in vitro. Xenobiotica 2022, 52, 435–441. [Google Scholar] [CrossRef] [Scilit]
- Leite, P.M.; Martins, M.A.P.; Carvalho, M.D.G.; Castilho, R.O. Mechanisms and interactions in concomitant use of herbs and warfarin therapy: An updated review. Biomed. Pharmacother. 2021, 143, 112103. [Google Scholar] [CrossRef] [Scilit]
- Vogel, J.H.; Bolling, S.F.; Costello, R.B.; Guarneri, E.M.; Krucoff, M.W.; Longhurst, J.C.; Olshansky, B.; Pelletier, K.R.; Tracy, C.M.; Vogel, R.A.; et al. Integrating complementary medicine into cardiovascular medicine. A report of the American College of Cardiology Foundation Task Force on Clinical Expert Consensus Documents (Writing Committee to Develop an Expert Consensus Document on Complementary and Integrative Medicine). J. Am. Coll. Cardiol. 2005, 46, 184–221. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Min, D.E.; Han, D.E.; Kang, K.; Ding, K.; Xu, G.; Lee, M.Y.; An, D.S.; Hur, N.; Kim, J.M.; Hong, J.Y.; et al. A comparative analysis of regulatory frameworks and their market impacts on health functional foods: Perspectives from South Korea, Canada, the United States, and China. Crit. Rev. Food Sci. Nutr. 2026, 1–24. [Google Scholar] [CrossRef] [Scilit]
- Shan, F.; Liu, L.; Li, L.; Wang, W.; Bi, Y.; Li, M. Management, Safety, and Efficacy Evaluation of Nutraceutical and Functional Food: A Global Perspective. Compr. Rev. Food Sci. Food Saf. 2025, 24, e70222. [Google Scholar] [CrossRef] [Scilit]
- Gupta, M.; Sharma, R.; Kumar, A. Docking techniques in pharmacology: How much promising? Comput. Biol. Chem. 2018, 76, 210–217. [Google Scholar] [CrossRef] [Scilit]
- Baig, M.H.; Ahmad, K.; Roy, S.; Ashraf, J.M.; Adil, M.; Siddiqui, M.H.; Khan, S.; Kamal, M.A.; Provazník, I.; Choi, I. Computer Aided Drug Design: Success and Limitations. Curr. Pharm. Des. 2016, 22, 572–581. [Google Scholar] [CrossRef] [Scilit]
- Yu, Z.; Wu, Z.; Wang, Z.; Wang, Y.; Zhou, M.; Li, W.; Liu, G.; Tang, Y. Network-Based Methods and Their Applications in Drug Discovery. J. Chem. Inf. Model. 2024, 64, 57–75. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wu, Z.; Li, W.; Liu, G.; Tang, Y. Network-Based Methods for Prediction of Drug-Target Interactions. Front. Pharmacol. 2018, 9, 1134. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Loscalzo, J. Molecular interaction networks and drug development: Novel approach to drug target identification and drug repositioning. FASEB J. 2023, 37, e22660. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, F.; Wen, Q.; Jiang, J.; Li, H.L.; Tan, Y.F.; Li, Y.H.; Zeng, N.K. Could the gut microbiota reconcile the oral bioavailability conundrum of traditional herbs? J. Ethnopharmacol. 2016, 179, 253–264. [Google Scholar] [CrossRef] [Scilit] [PubMed]



| Herb | Major Bioactive Components | Main Chemical Structure | Primary Cardiovascular Activities |
|---|---|---|---|
| Hawthorn fruit | Hyperoside, ursolic acid | 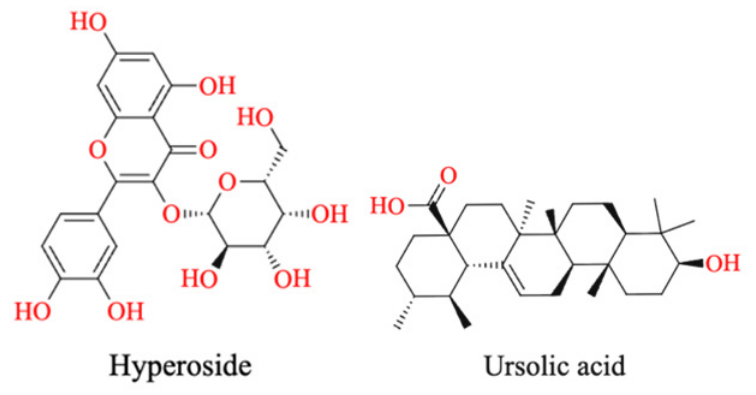 | Antioxidant, lipid regulation, inhibits LDL oxidation, inhibits HMG-CoA reductase, activates Nrf2 |
| Ginkgo seed | Ginkgetin, ginkgolide B |  | Antioxidant, anti-inflammatory, anti-PAF, neuroprotection |
| Milkvetch root | Astragaloside IV |  | Improves endothelial function, anti-fibrosis |
| Turmeric | Curcumin |  | Anti-inflammatory, antioxidant |
| Ginger | 6-Gingerol |  | Antioxidant, anti-inflammatory, antiplatelet |
| Glossy ganoderma | Ganoderic acid A |  | Lipid regulation, anti-inflammatory |
| Angelica sinensis | Ferulic acid, ligustilide |  | Antithrombotic, vasodilation, antiplatelet |
| Barbary wolfberry fruit | Zeaxanthin |  | Antioxidant, anti-LDL oxidation |
| Lotus leaf | Nuciferine |  | Lipid regulation and weight loss, antiarrhythmic |
| Honey | Quercetin |  | Antioxidant, anti-LDL oxidation |
| Medicinal Cuisine Name | Competition and Preparation | Traditional Functions | Target Population | Modern Mechanistic Research |
|---|---|---|---|---|
| Hawthorn fruit–lotus leaf lipid-regulating tea | Dried hawthorn fruit 10 g, dried lotus leaf 6 g; steep in boiling water or decoct for 15 min | Promotes digestion and resolves accumulation, raises the clear and lowers the turbid | Hyperlipidemia, pre-obesity | Hawthorn fruit flavonoids inhibit cholesterol synthesis; nuciferine activates AMPK |
| Milkvetch root–Angelica sinensis stewed chicken | Milkvetch root 30 g, Angelica sinensis 10 g, chicken 500 g; stew for 1.5 h | Tonifies qi and nourishes the blood, invigorates the blood and unblocks collaterals | Qi-blood deficiency type, postoperative recovery | Astragaloside IV improves endothelial function; ferulic acid is antithrombotic |
| Glossy ganoderma–Poria spirit-calming congee | Glossy ganoderma powder 3 g, Poria 15 g, polished rice 100 g; cook as congee | Calms the heart and spirit, strengthens the spleen and promotes diuresis | Insomnia, anxiety, low immunity | Glossy ganoderma polysaccharides provide immunomodulation; triterpenes are anti-inflammatory |
| FMC Substance | Major Bioactive Compounds | Lipid Regulation | Anti- Inflammation | Endothelial Protection | Anti- Oxidant | Gut Microbiota Modulation | Highest Level of Clinical Evidence |
|---|---|---|---|---|---|---|---|
| Hawthorn fruit | Hyperoside, ursolic acid, procyanidin B2 | ++ (animal) | + (in vitro) | + (animal) | ++ (in vitro/animal) | – | Meta-analyses of RCTs (heart failure symptoms; no AS endpoints) |
| Ginkgo seed | Ginkgolides, bilobalide, biflavonoids | + (in vitro) | ++ (animal) | ++ (in vitro/animal) | ++ (in vitro/animal) | – | No AS-specific RCTs |
| Milkvetch root | Astragaloside IV, calycosin | + (animal) | + (in vitro/animal) | +++ (in vitro/animal) | + (in vitro) | – | Small observational studies only (Chinese language) |
| Turmeric | Curcumin | + (animal) | +++ (in vitro/animal) | + (in vitro) | +++ (in vitro/animal) | + (animal) | Limited RCTs (biomarkers only; no AS endpoints) |
| Ginger | 6-Gingerol, 6-shogaol | + (animal) | ++ (in vitro/animal) | + (in vitro) | ++ (in vitro/animal) | – | Meta-analyses supporting BP, TG, LDL-C reduction |
| Glossy ganoderma | Ganoderic acid A, β-glucans | ++ (animal) | ++ (in vitro/animal) | – | + (in vitro) | ++ (animal) | Cochrane review: no effect on CV risk factors (3 RCTs in T2DM) |
| Angelica sinensis | Ferulic acid, ligustilide | – | + (in vitro) | ++ (in vitro/animal) | + (in vitro) | – | No AS-specific clinical trials |
| Barbary wolfberry fruit | Zeaxanthin, LBP | – | + (in vitro) | – | ++ (in vitro/animal) | – | No AS-specific clinical trials |
| Lotus leaf | Nuciferine, RG-I pectin | ++ (animal) | – | – | – | ++ (animal, FMT confirmed) | No AS-specific clinical trials |
| Honey | Quercetin, phenolic acids | + (clinical) | + (in vitro) | – | ++ (in vitro/clinical) | – | Meta-analysis (conflicting results on lipids) |
| Herb | Risk Mechanism | Specific Manifestations | High-Risk Populations/Drugs |
|---|---|---|---|
| Ginkgo semen | Ginkgotoxin, anti-PAF, antiplatelet aggregation | Tonic–clonic seizure, prolonged bleeding time | Patients with epilepsy; heavy consumers; warfarin, aspirin, clopidogrel users |
| Ginger | High dose (>4 g/day) inhibits platelets | Increased bleeding risk | Perioperative period, anticoagulation therapy patients |
| Glossy ganoderma | Immunomodulatory effects | Adverse event risk increased 1.67-fold (non-serious) | Post-organ transplant (immunosuppressant users); active autoimmune disease |
| Hawthorn fruit | Positive inotropic effect, vasodilation | May enhance vasodilator and digoxin effects | Heart failure patients with LVEF ≤ 35%; digoxin users |
| Turmeric | High dose inhibits platelet aggregation; inhibits CYP3A4/2C9 | Theoretically increases bleeding risk; affects drug metabolism | Anticoagulation therapy patients, perioperative period; statin users |
| Barbary wolfberry fruit | Immune activation; may enhance warfarin effects | Active autoimmune disease risk; elevated INR | Active systemic lupus erythematosus, rheumatoid arthritis; warfarin users |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.
Share and Cite
Zhang, X.; Dong, M.; Wang, X.; Hong, Y.; Zhang, X.; Niu, Y.; Li, X. Bioactive Constituents, Mechanisms, and Complementary Therapeutic Applications of Food–Medicine Continuum Materia Medica for Atherosclerosis Prevention and Treatment. Pharmaceuticals 2026, 19, 856. https://doi.org/10.3390/ph19060856
Zhang X, Dong M, Wang X, Hong Y, Zhang X, Niu Y, Li X. Bioactive Constituents, Mechanisms, and Complementary Therapeutic Applications of Food–Medicine Continuum Materia Medica for Atherosclerosis Prevention and Treatment. Pharmaceuticals. 2026; 19(6):856. https://doi.org/10.3390/ph19060856
Chicago/Turabian StyleZhang, Xiaorong, Mengyue Dong, Xinke Wang, Yingjie Hong, Xin Zhang, Yonghuan Niu, and Xuefeng Li. 2026. "Bioactive Constituents, Mechanisms, and Complementary Therapeutic Applications of Food–Medicine Continuum Materia Medica for Atherosclerosis Prevention and Treatment" Pharmaceuticals 19, no. 6: 856. https://doi.org/10.3390/ph19060856
APA StyleZhang, X., Dong, M., Wang, X., Hong, Y., Zhang, X., Niu, Y., & Li, X. (2026). Bioactive Constituents, Mechanisms, and Complementary Therapeutic Applications of Food–Medicine Continuum Materia Medica for Atherosclerosis Prevention and Treatment. Pharmaceuticals, 19(6), 856. https://doi.org/10.3390/ph19060856