Article

Genetic Investigations on the Sicilian Populations of Prunus mahaleb L. and Prunus cupaniana Guss ex E. Huet & A. Huet (Rosaceae): Implications for Conservation


1
Research Institute on Terrestrial Ecosystems, National Research Council, Via Marconi 2, 05010 Porano, Italy
2
Institute of Biosciences and Bioresources, National Research Council, Via La Malfa 153, 90146 Palermo, Italy
3
Department of Agricultural, Food and Forest Sciences, University of Palermo, Viale delle Scienze, Edificio 4, 90128 Palermo, Italy
*
Author to whom correspondence should be addressed.
Diversity 2026, 18(7), 438; https://doi.org/10.3390/d18070438
Submission received: 22 June 2026 / Revised: 14 July 2026 / Accepted: 17 July 2026 / Published: 21 July 2026
(This article belongs to the Section Plant Diversity)

Abstract

Assessing genetic diversity of species and populations can help reduce the risk of biodiversity loss by identifying areas deserving the greatest attention in terms of conservation priority. Our study was focused on evaluating the genetic variability of Prunus mahaleb L. and Prunus cupaniana Guss. ex E. Huet & A. Huet (Rosaceae), both of which are quite rare and unevenly distributed in Sicily (Italy). In this region, P. mahaleb occurs in scattered populations, mostly concentrated on the mountain ranges close to the northern Tyrrhenian coast, while P. cupaniana, which is endemic in Sicily, is known to occur only on Sicani Mountains and on the Madonie Massif. A total of 118 georeferenced individuals of P. mahaleb and P. cupaniana were sampled across eight different sites. The samples were genotyped using nine unlinked nSSr loci. A high percentage of clonal individuals was observed especially in P. cupaniana. Low intrapopulation diversity, as well as high divergence among populations were recorded. The analysis performed using STRUCTURE separated P. mahaleb and P. cupaniana into two different gene pools (K = 2) and revealed the complete absence of introgression between them. These results, if confirmed through further molecular analysis, indicate that these taxa should be considered as two distinct species. Moreover, more detailed analyses allowed us to distinguish four gene pools for P. mahaleb, while the extant populations of P. cupaniana could be grouped into two clusters suggesting their strong isolation and a very low, if any, absent gene flow between them. Our results underline the urgent need for interventions aimed at conserving and managing the genetic heritage of the Sicilian populations of both species.

1. Introduction

The amount of genetic diversity represents an important indicator of biodiversity and is widely recognized as the key component for the long-term survival of species [1]. Genetic diversity provides the raw material for adaptation and evolution, especially under rapidly changing environmental and disease pressures [2]. Hence, studies assessing levels of genetic diversity can help reduce the risk of biodiversity loss by identifying the populations and areas showing the highest values of genetic variability and deserving the most attention in terms of conservation priority [3]. In situ and ex situ conservation plans must consider the intraspecific genetic variation as a fundamental criterion for developing effective conservation strategies [4,5]. Several surveys have highlighted the enormous value of the genetic heritage of Sicilian forests [6]. Despite covering only about 10% of the island, local woodlands host the richest tree flora in Italy. Many woody species have here the southernmost edge of their distribution range. In many cases they may have developed adaptations to extreme environmental conditions, making Sicilian populations of paramount interest for reforestation activities in an increasingly alarming scenario of global warming.
In this context, our study focused on evaluating the genetic variability of Prunus mahaleb L. and Prunus cupaniana Guss. ex. Huet & A. Huet, two woody taxa belonging to the genus Prunus (Rosaceae), in order to support the implementation of management and conservation measures for the Sicilian forests.
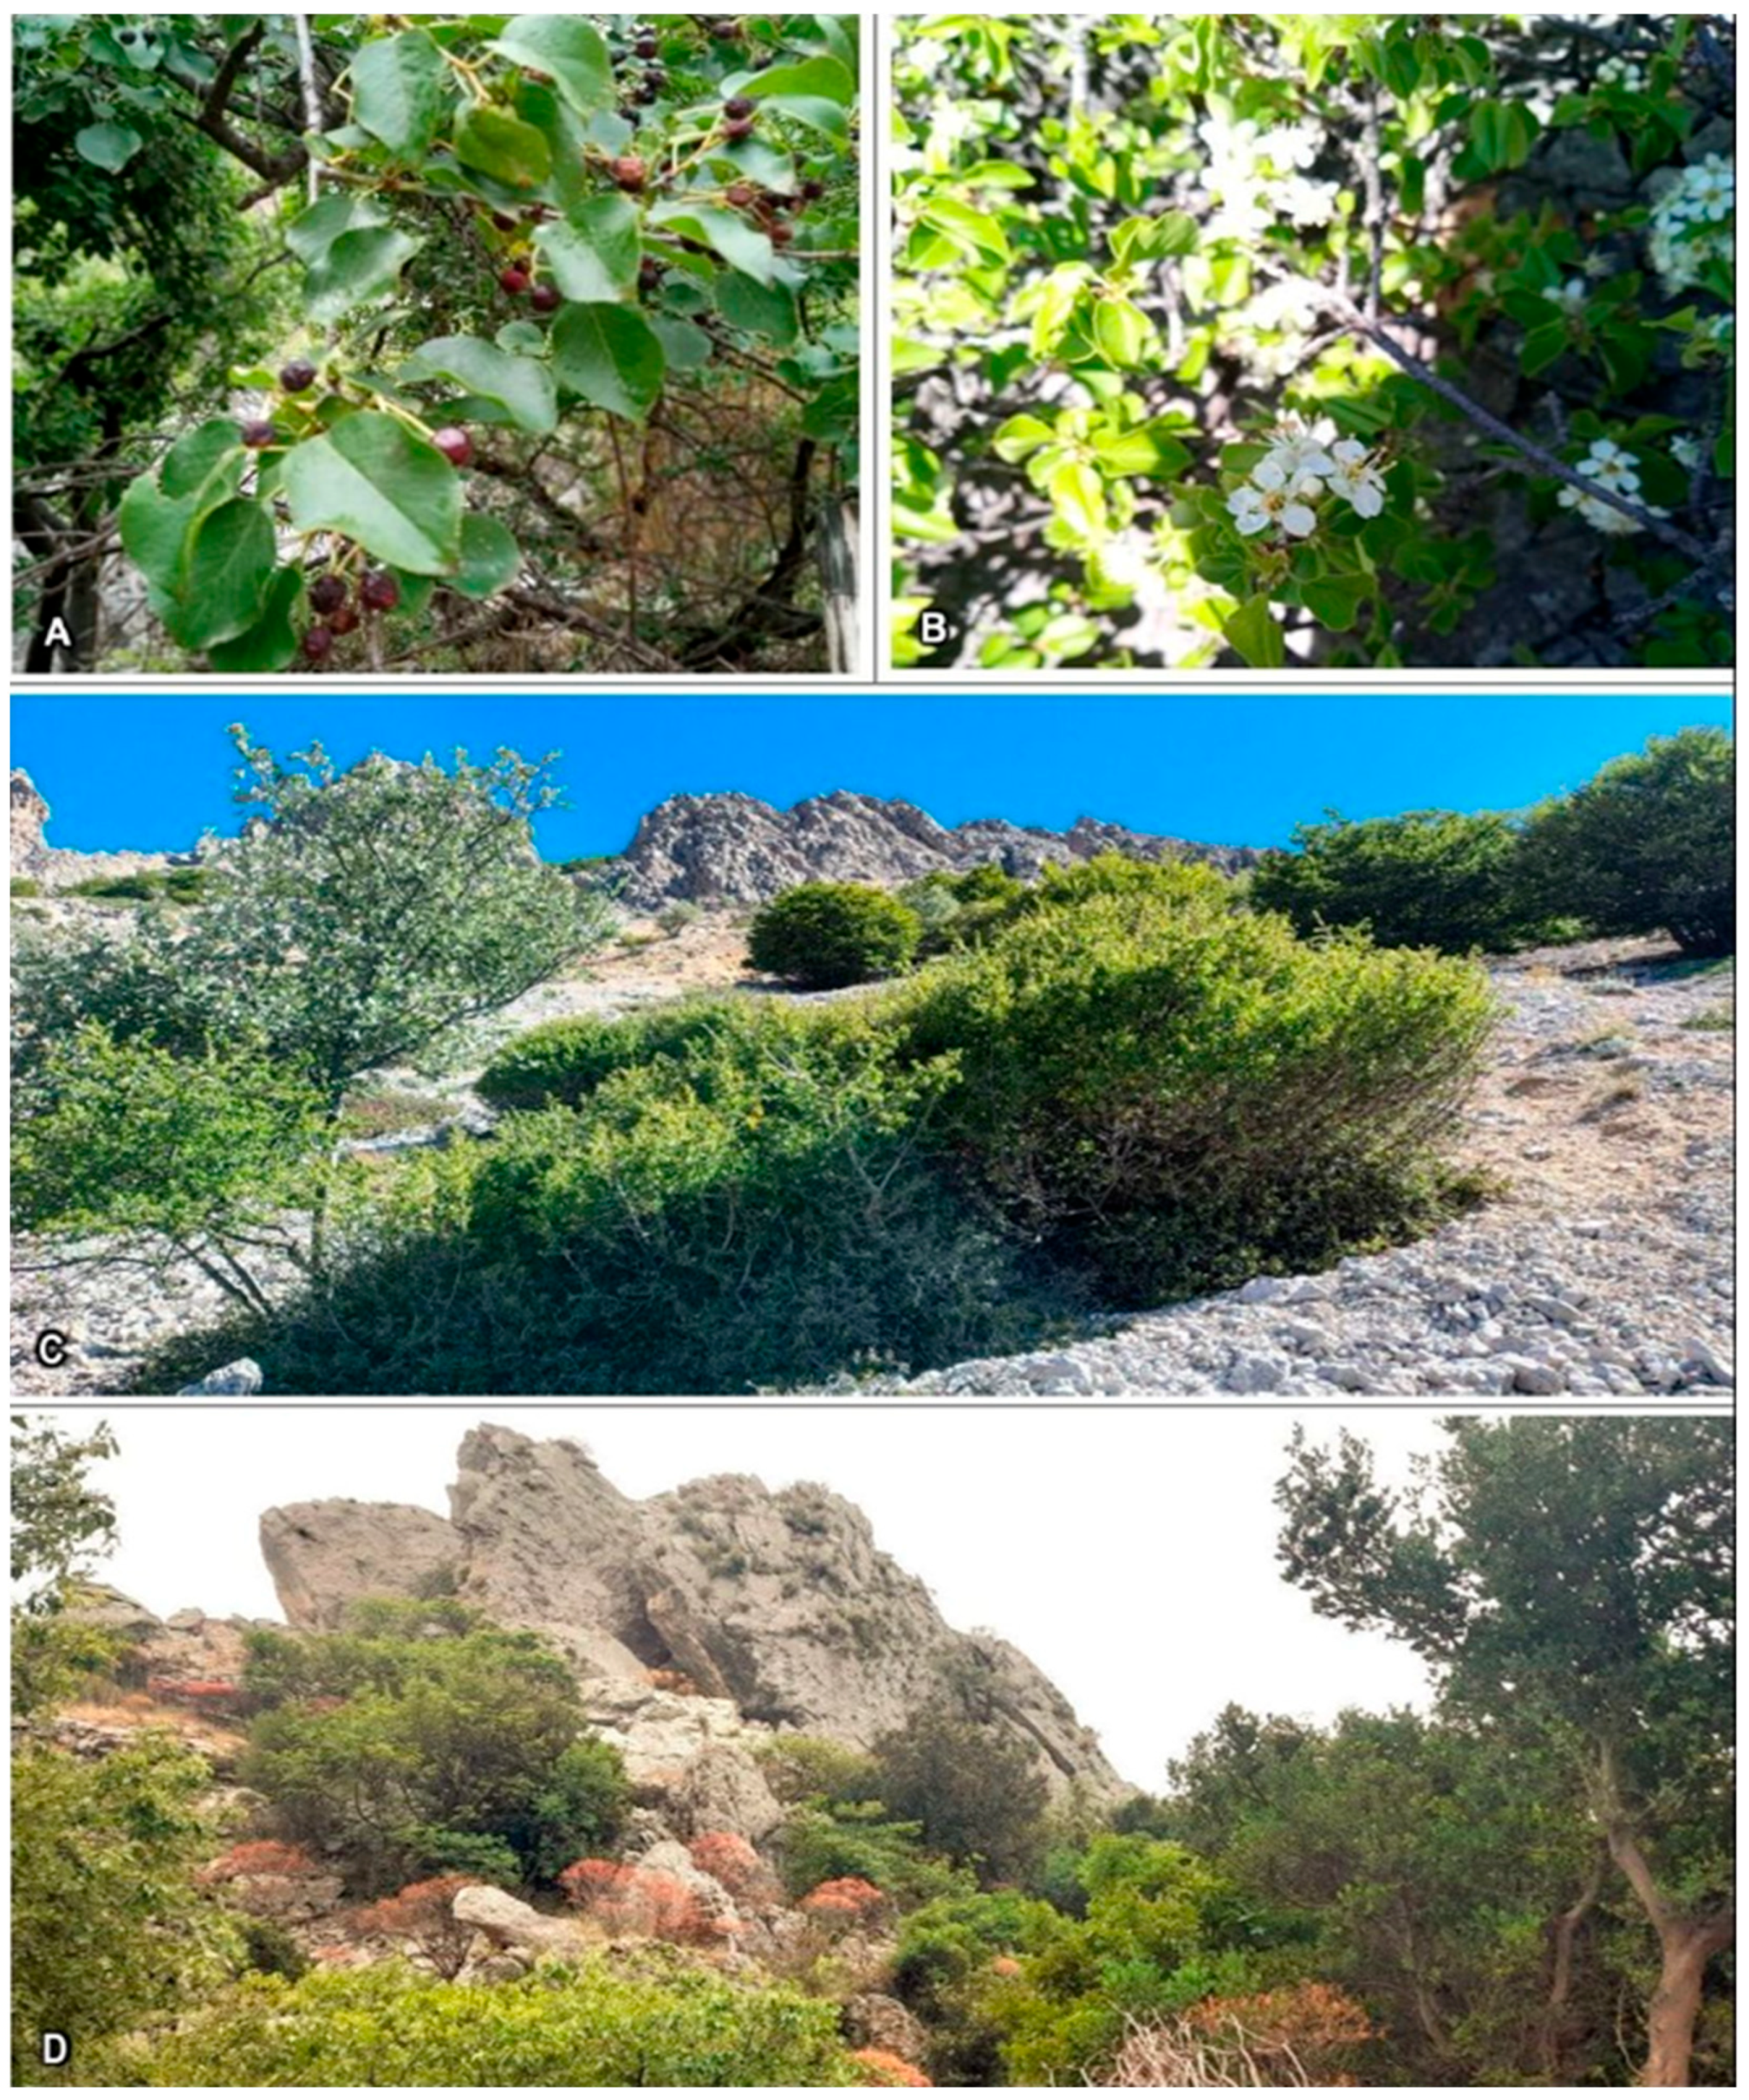
P. mahaleb, known as mahaleb cherry or St. Lucie’s cherry, is a deciduous shrub or small tree, up to 10 (max 15) m tall (Figure 1A). Its bark is dark brown, smooth, and glossy [7]. The leaves are alternate, 4–7 cm long, broadly ovate, pointed, base rounded to almost cordate; its margins are finely saw-toothed with marginal glands, glossy above and slightly hairy along the midrib beneath [7]. It is a relatively long-lived species compared to its closest relatives (i.e., P. avium L., the sweet cherry tree, and P. cerasus L., the sour cherry tree). Due to its extensive root system and its pioneer behaviour, P. mahaleb has long been used in horticulture as frost resistant rootstock for both P. avium and P. cerasus [8,9,10]. The natural range of P. mahaleb stretches from Central and Southern Europe towards the Middle East (Lebanon and Syria) [11,12,13]. It occurs in almost all the regions of the Italian Peninsula but is relatively rare in the western regions and shows a very fragmented and discontinuous distribution pattern throughout the central-northern Apennines, with very isolated populations in the rest of southern Italy [14].
In Sicily, P. mahaleb occurs in several scattered populations, mostly concentrated in the mountainous areas close to the northern Tyrrhenian coast, in the Mts. of Trapani and Palermo and in Sicani Mts., whereas it is absent in the Madonie Massif. It also grows on the southern and eastern slopes of Nebrodi Mts. (Figure S1) while on the Peloritani Mts. it is only reported to grow along the catchment of the river Mela [15]. Its historical presence on Mt. Etna, documented by herbarium specimens, has not been confirmed recently.
Prunus cupaniana (Figure 1B) is known to occur only in the territory of Sicani Mts. (Ficuzza-Rocca Busambra) and on the Madonie Massif [16] (Figure S1). This narrow-ranged endemism was first suspected to be a distinct species by Gussone [17,18], then included within the variability of P. mahaleb and treated as a subspecies by Arcangeli [19], Pénzes [20], and Soják [21] up to recent times [16,22], while Nyman [23], Lojacono-Pojero [24] and Fiori [25,26]) considered P. cupaniana just a variety or even as a ‘proles ’ [27] or mountain ecotype. It differs from P. mahaleb in its prostrate or ascending, multi-stemmed bushy habit, leathery leaves with cordate and smaller lamina and corymbs with fewer flowers bearing smaller petals [16]. Moreover, the existence of distinct vernacular names, i.e., “Ciràsa lampàsa” or “Ciràsa purganti” for P. mahaleb, “Amarèni di muntagna” for P. cupaniana, attests to the fact that they were already recognized as different taxa by Sicilian people and botanists in the early 18th century [28].
The taxonomic interpretation of P. cupaniana remains controversial and, to the best of our knowledge, until now, it is mostly based only on morphological characters, while no detailed molecular data is available to date.
The principal goals of our work were:
(1)
To perform genetic analysis based on microsatellite markers to assess the genetic diversity and divergence of the extant Sicilian populations of P. mahaleb and P. cupaniana.
(2)
To evaluate the genetic distance between these two taxa and the possible occurrence of hybrids where they co-exist.
Based on our results, we aim to provide guidance on the management and conservation of these precious genetic resources.

2. Materials and Methods

2.1. Plant Material

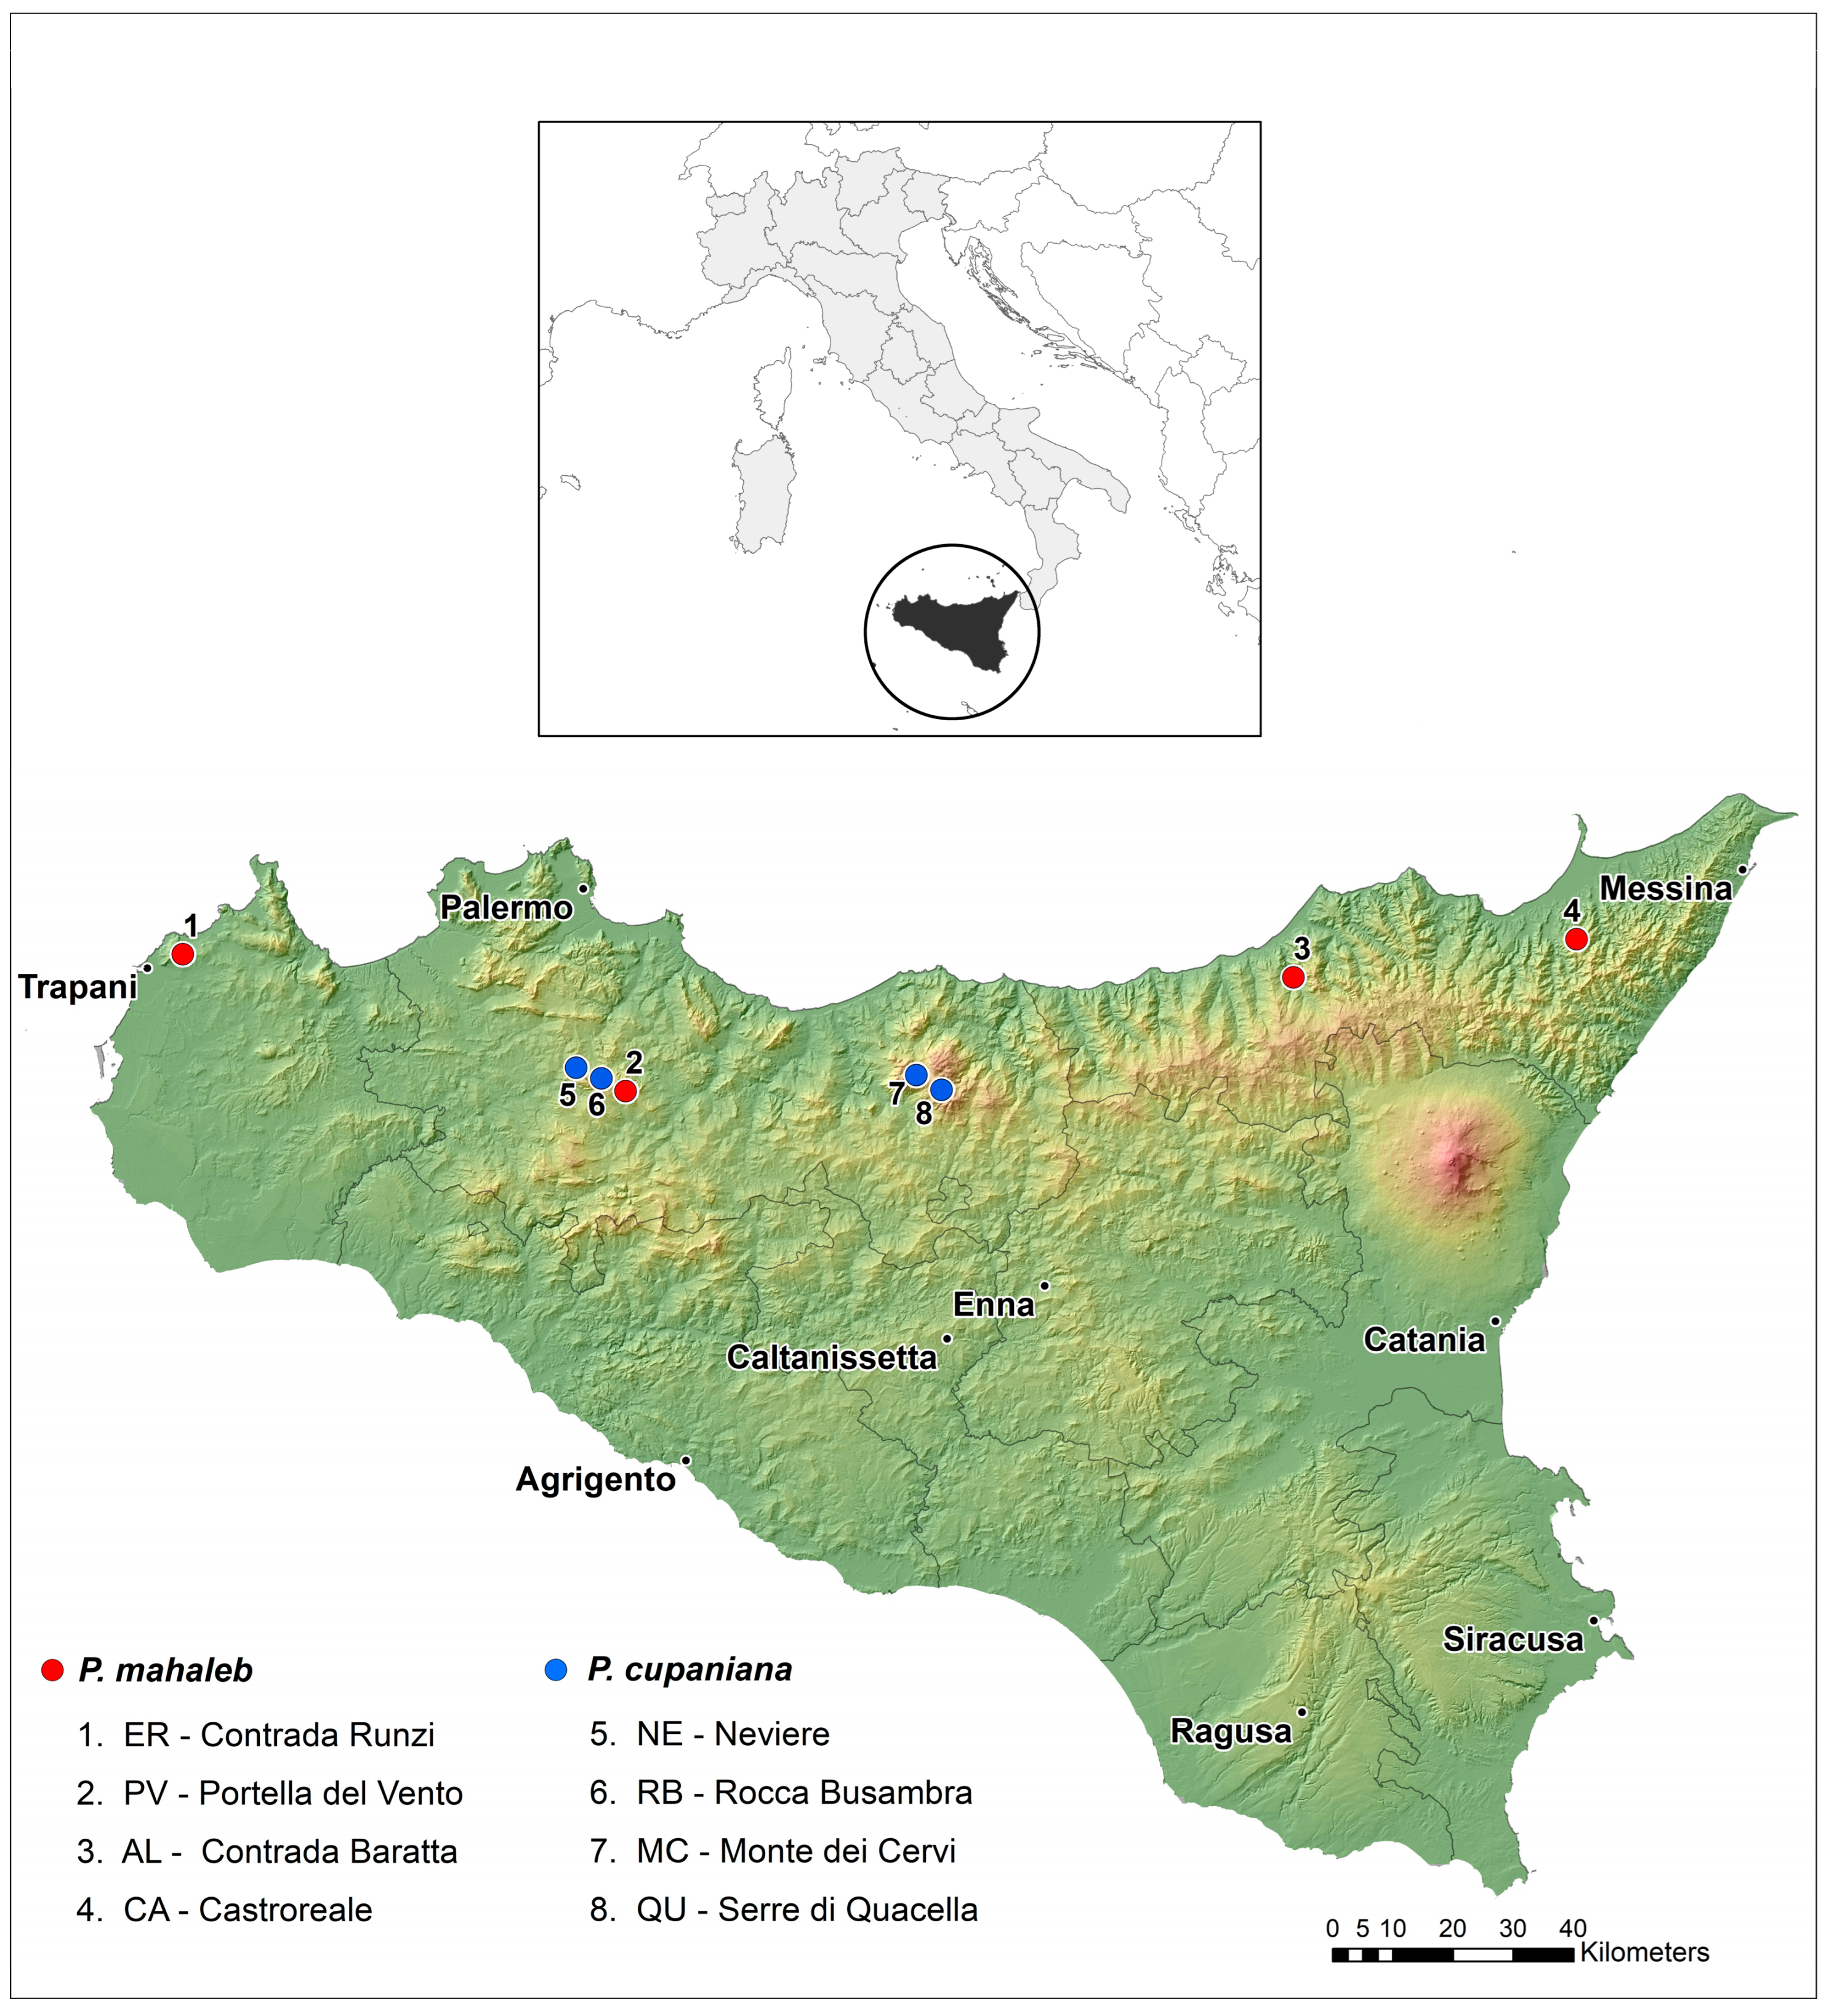
To define the optimal sampling grid for plant material, the regional distribution range of Prunus mahaleb and Prunus cupaniana was first delineated [15] (Figure S1). To this end, data was drawn from the scientific literature, from the working group’s own observations, as well as from information provided by local experts. All this distribution data was compiled into a geodatabase. We recorded a larger distribution area for P. mahaleb on Trapani Mts, Sicani Mts, Nebrodi and Peloritani Mts., while P. cupaniana was recorded only on Sicani and Madonie Mts. Sampling was carried out between autumn 2023 and spring 2024 (Figure 2), except for RB and QU stands, where material was collected in autumn 2025. A total of 118 georeferenced individuals of P. mahaleb and P. cupaniana were sampled in 8 populations located in seven different Sicilian geographical areas. All the sampling sites fall within the natural distribution range of the target taxa (Figure S1), and some of them are located in protected areas such as regional nature reserves or parks (Table 1 and Figure 2). Three sites only hosted P. mahaleb on Trapani Mts. (ER) on Nebrodi Mts. (AL) and on Peloritani Mts., (CA), two sites in the Madonie Mts. only P. cupaniana (MC, QU). The two taxa coexisted on the Sicani Mts. Nature Reserve Bosco della Ficuzza, Rocca Busambra, in this area we sampled P. cupaniana in two sites (RB, NE) and P. mahaleb in one stand (PV).
An ecological analysis of the stands was conducted to assess site-specific abiotic and ecological (altitude, aspect, habitat type, threats) as well as biotic (vegetative status, growth habit, consistency of flowering and fruiting, regeneration, and phytosanitary status) parameters (Table 1). Furthermore, each stand was classified following the official inventory of the regional Forest Types [29]. Within each stand, leaf material was collected from a minimum of 6 and a maximum of 20 healthy trees located (when possible) almost 15–20 m apart. A minimum of 20 young leaves were collected from each tree and stored at −20 °C for DNA extraction and analysis.
Due to the small and uneven number of individuals present on the sites, it was not always possible to collect individuals distant enough to minimize the sampling of close relatives. To overcome this problem, subsequent genetic analysis allowed us to discard clonal individuals.

2.2. DNA Isolation, SSRs Amplification and Genotyping

Leaf tissues (50 mg) from each sample were homogenized in a 2 mL microcentrifuge tube containing 5 mm-long steel beads cooled with liquid nitrogen using Mixer Mill 300 (Qiagen, Hilden, Germany). Genomic DNA was extracted and purified using a DNeasy 96 plant kit (Qiagen) and stored at −20 °C. The samples were then genotyped using 9 unlinked nSSr loci EMPaS12, EMPaS02, EMPaS06, EMPaS14 [30] UDP96-005, UDP98-412, UDP97-402 [31], and PceGA34 PS1202 [32]. The genetic linkage of the loci was investigated in Prunus mapping progenies and all were proved to be unlinked [30,31]. Three multiplex PCRs were set up based on the size of products, using fluorescent dye-labelled primers (6-FAM, VIC, NED, PET; Applied Biosystems, Foster City, CA, USA). Amplifications were performed with the Type-It Microsatellite PCR Kit (Qiagen, Valencia, CA, USA).
The PCR reactions were performed in 12.5 µL total volume containing 20 ng of genomic DNA. Amplification conditions were as follows: an initial step at 95 °C for 5 min, followed by 27 cycles at 95 °C for 30 s, 57 °C for 1.5 min, and 72 °C for 30 s. A final extension step at 60 °C for 30 min was executed. PCR fragments have been run on a SeqStudio TM Genetic Analyzer (ThermoFisher Scientific, Waltham, MA, USA) for separation and sizing. GeneScan250 LIZ (ThermoFisher Scientific, Waltham, MA, USA) was used as an internal size standard. Genotyping was performed using GeneMapper v4.0 software (ThermoFisher Scientific).

2.3. Genetic Diversity and Structure of Prunus Populations

The clonal individuals were identified for each population using the “Multilocus Matches Parameters” analysis of GenAlEx 6.5 software [33] and were removed from the raw data. All subsequent statistical analyses were performed using unique genotypes. The genetic diversity of each population was also performed with GenAlEx 6.5 software [33]; the mean number of alleles per locus (Ne), observed (Ho) and expected heterozygosity (He), heterozygosity corrected for sample size (UHe), Shannon Index (I) and fixation index (Fis) were calculated. Allelic richness (Ar) was evaluated with HP-Rare 1.0 software [34]. The AMOVA analysis was performed using the software GenAlEx 6.5.
To assess the genetic differentiation between the analyzed Prunus populations two approaches were adopted, i.e., (1) Principal Coordinate Analysis (PCoA), performed with GenAlEx 6.5 software, (2) Bayesian clustering implemented in STRUCTURE 2.3.3 software [35]. For this last analysis, the range of possible number of clusters (K) tested was equal to the number of the populations analyzed plus one. Parameters were set for a burn-in period of 100,000 and a MCMC (Markov chain Monte Carlo) with 200,000 iterations. Potential clusters (K) were tested using 10 iterations. To determine the most likely number of K, the ΔK method by Evanno et al. [36] was applied using STRUCTURE HARVESTER [37]. The groups indicated by the STRUCTURE 2.3.3 analysis were subsequently analyzed separately to identify subgroups within each cluster.

3. Results

By performing the “Multilocus Matches” analysis using the GenAlEx 6.5 software, we could identify the presence of several clonal individuals, mostly belonging to the Prunus cupaniana populations (Table S1). From the initial 118 individuals we obtained 93 unique genotypes, 52 samples of Prunus mahaleb and 41 samples of P. cupaniana. The highest number of clonal individuals were found in Prunus cupaniana populations (NE, QU, RB) (Table S1). All subsequent analyses were performed using only one individual representing each clonal genotype.

3.1. Genetic Diversity

In this study, P. mahaleb showed higher genetic diversity average values compared with P. cupaniana. In Table 2, the mean values of genetic indices are reported. A higher number of effective alleles (Ne = 4.17) was observed for the P. mahaleb samples compared with those of P. cupaniana (Ne = 2.71). A similar trend was recorded considering the heterozygosity observed (Ho, P. mahaleb = 0.524, P. cupaniana = 0.244), the expected (He, mahaleb = 0.735, cupaniana = 0.479) and the unbiased (uHe, P. mahaleb = 0.742, P. cupaniana = 0.485). The Shannon Index diversity (I) was 1.63 for P. mahaleb and 0.964 for P. cupaniana. A higher inbreeding coefficient (Fis) was observed for the P. cupaniana samples (Fis = 0.438), pointing at an excess of homozygotes. The genetic diversity indices were also calculated by a single population (Table 3). Overall, the populations of P. mahaleb showed higher values of genetic diversity compared to populations of P. cupaniana. The highest values of Shannon Diversity Index (I) and observed (Ho), expected (He) and unbiased (uHe) heterozygosity were recorded in the CA population of P. mahaleb. This population also showed the highest values of allelic richness (Ar) and private allelic richness (PAr). On the other hand, lower values of these parameters were observed in the populations of P. cupaniana, especially in the NE population (Ho = 0.22, uHe = 0.11).
All the populations of P. cupaniana showed positive values of inbreeding coefficient (Fis), while the differentiation among populations (Fst) is comparable for both taxa.

3.2. Population Structure

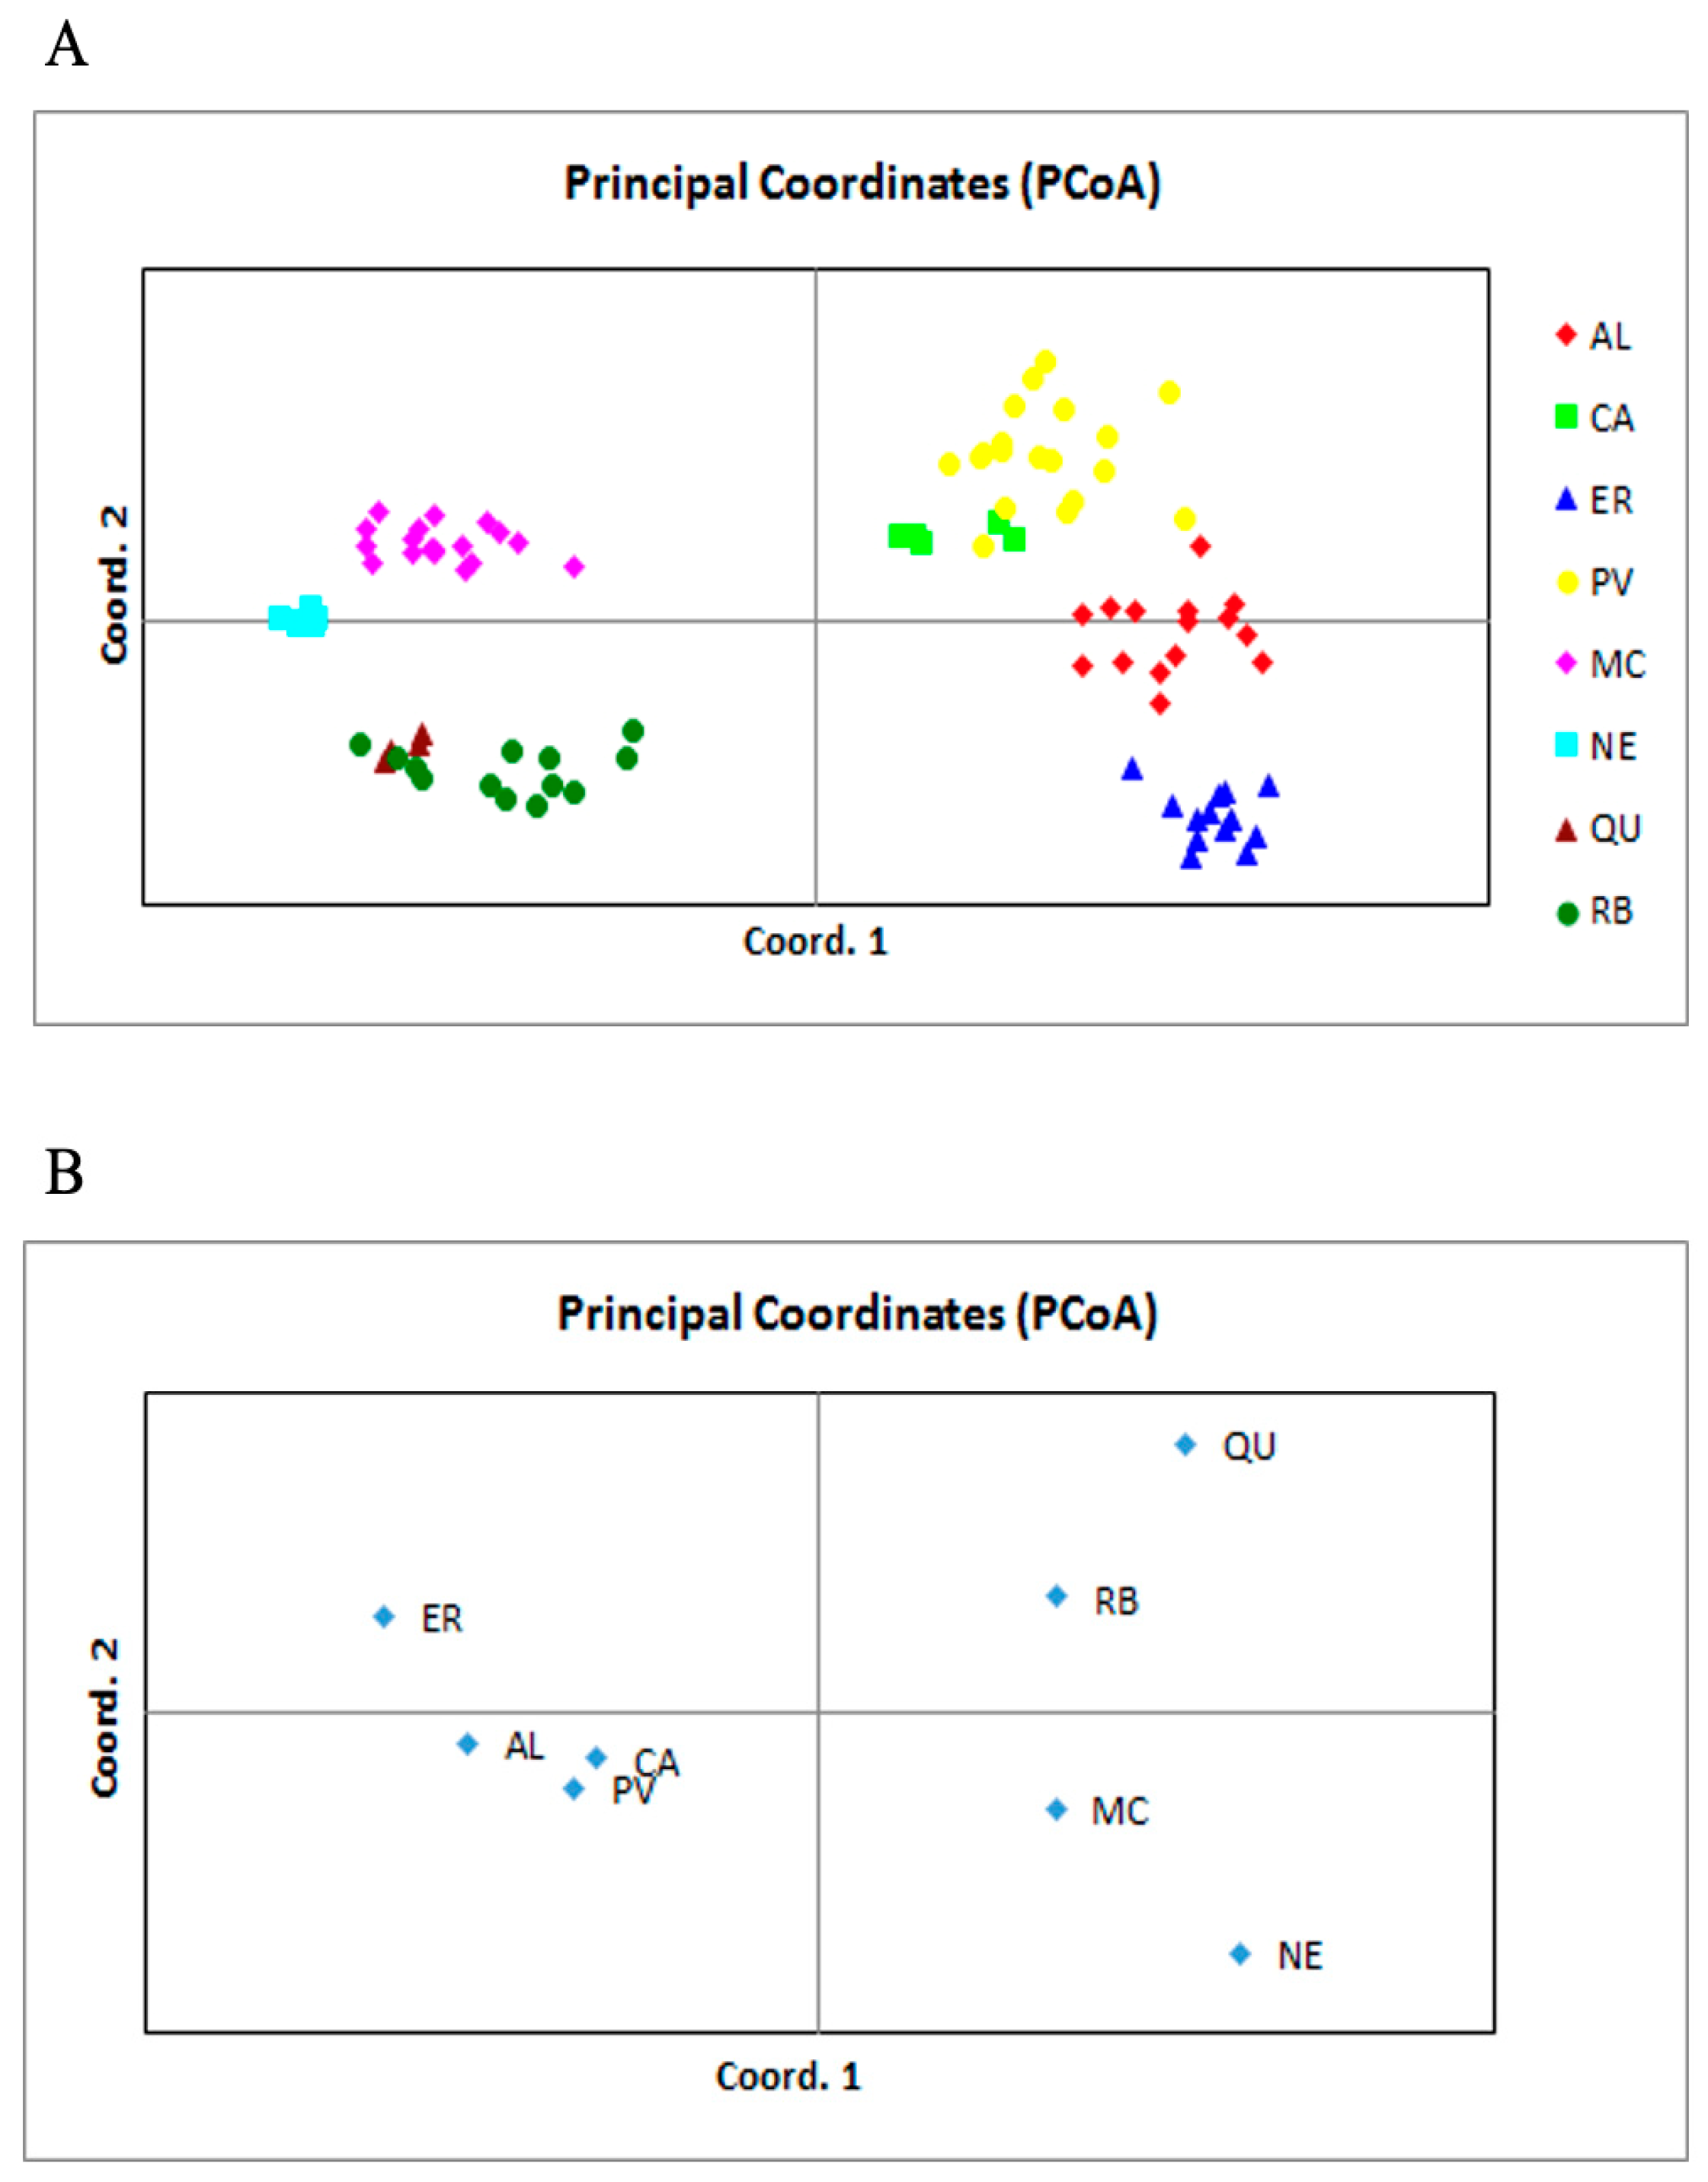
The PcoA analysis was performed considering the matrix of genetic distance (GD GeneAlEx) among all individuals of both P. mahaleb and P. cupaniana (Figure 3A). Then individuals were grouped into populations and the Fst matrix among populations was used to perform PcoA analysis (Figure 3B). Both the analyses pointed at the presence of a non-random clustering of individuals/populations.
Figure 3A shows the PcoA among individuals; the combination of the first two axes explained 38.97% of the variation. In the PcoA, performed using the Fst distance among populations (Figure 3B), 55.54% of the variance was explained by combining the variation in the first two axes.
In both Figure 3A,B, two main groups could be easily distinguished, suggesting a clear separation between the populations of P. cupaniana and P. mahaleb and highlighting the genetic divergence between these two taxa. In addition, the analysis of AMOVA indicated a high value variance (52%, p < 0.001) among P. cupaniana and P. mahaleh populations. Among the populations of P. cupaniana we observed a variance value of 41% (p < 0.001), while 38% (p < 0.001) of variance was recorded among the populations of P. mahaleb.
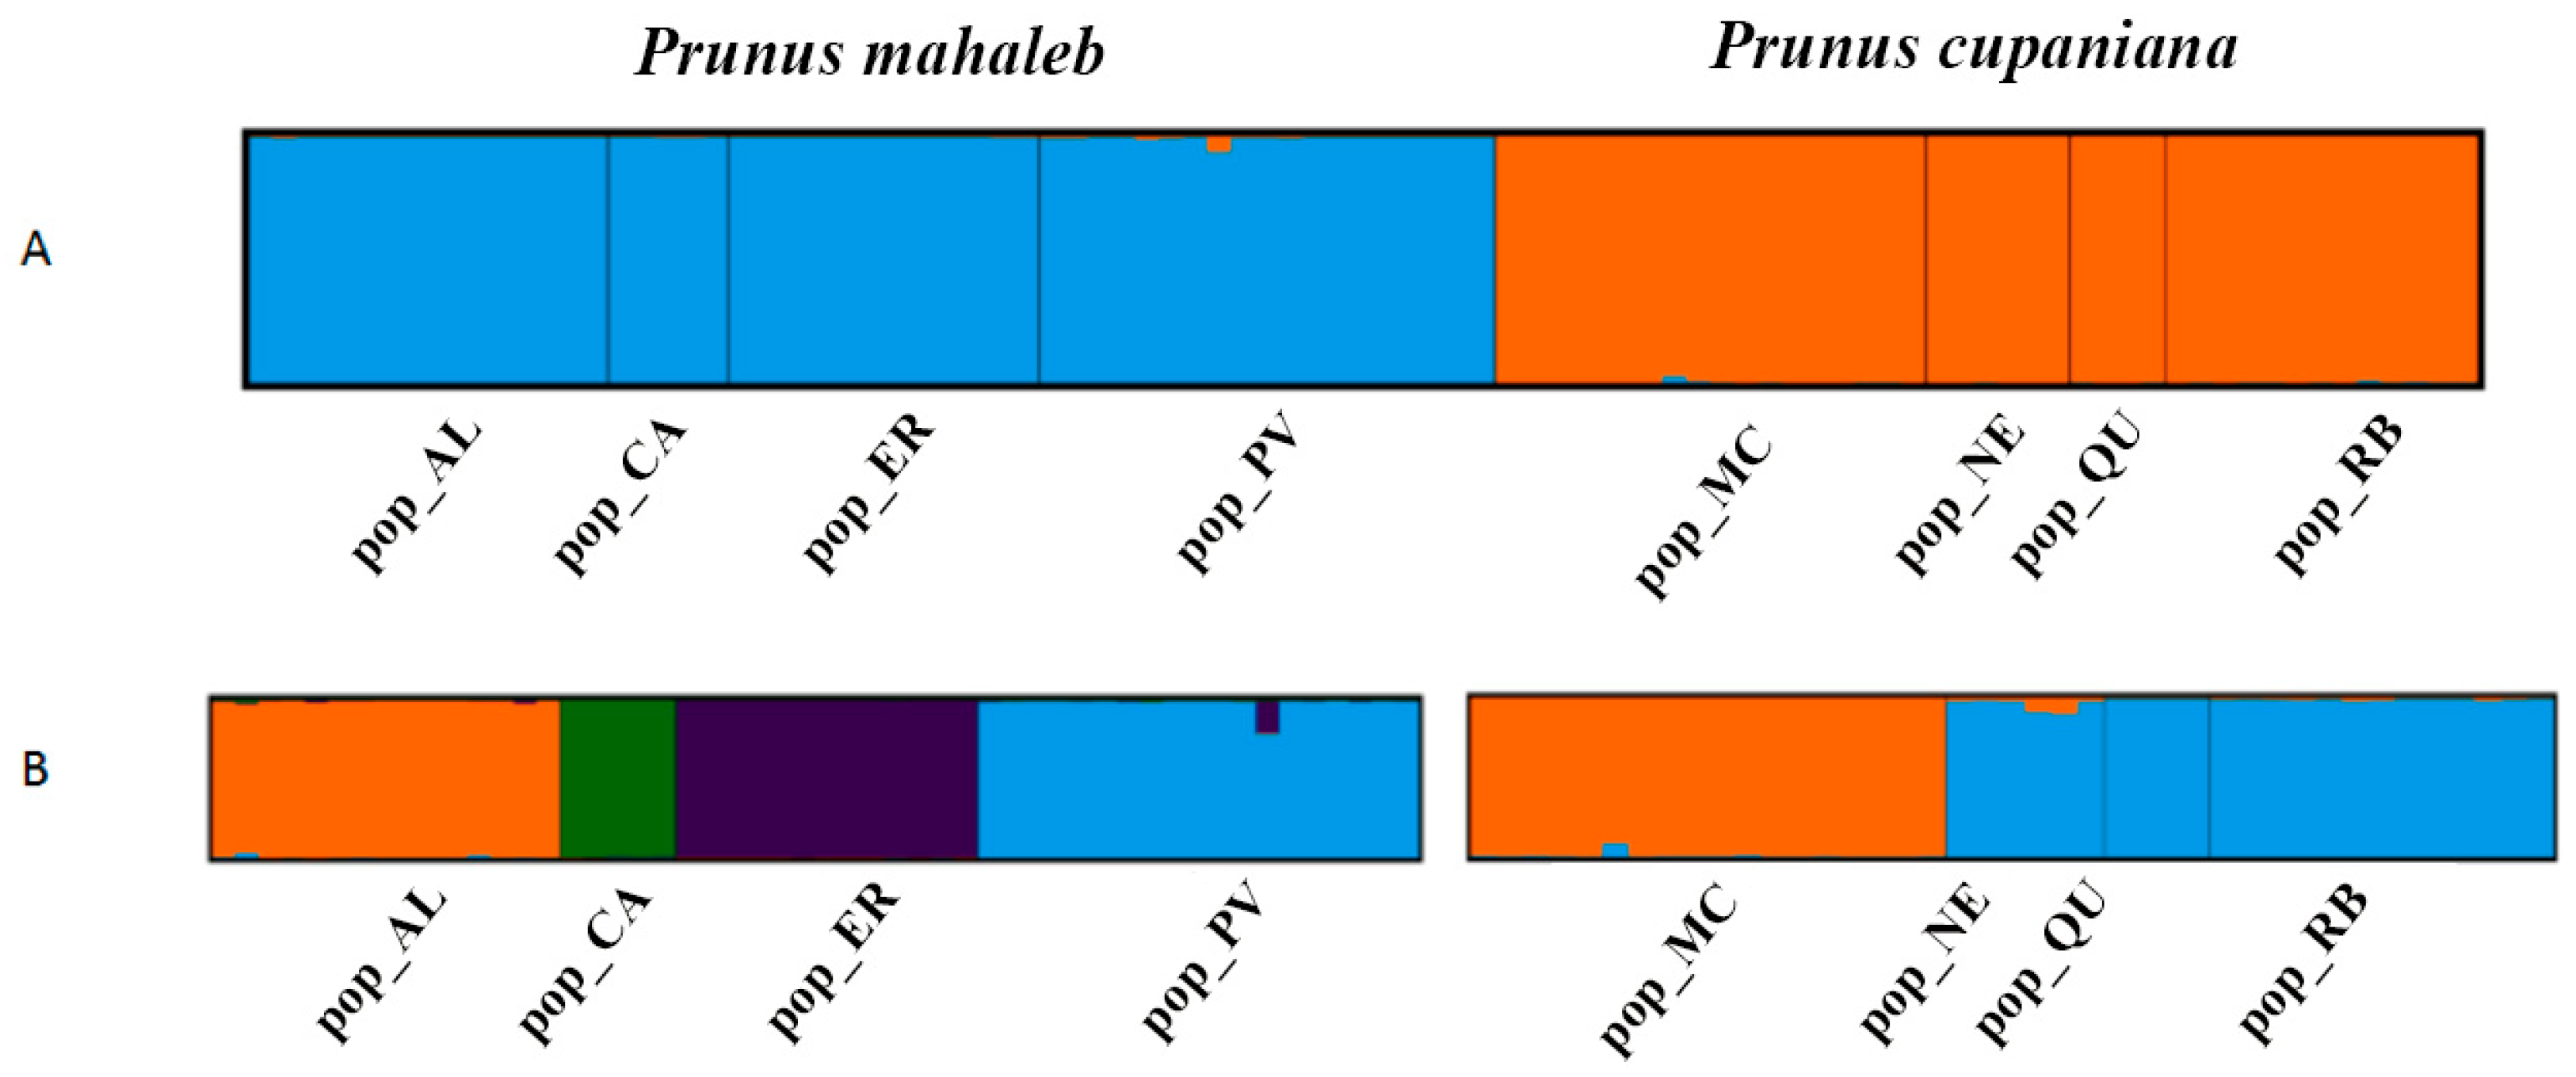
The subsequent STRUCTURE analysis corroborated the PCoA results. The most probable division among the populations belonging to the P. cupaniana and P. mahaleb, with stronger support in terms of log-likelihood, was detected at K = 2 (Figure 4).
The high values of Delta K recorded pointed at the sharp genetic distinctness of the two taxa (Figure 4A). It is worth emphasizing the total absence of introgressed individuals even in the Sicani Mts. locations (populations PV, RB and NE) where the two taxa co-exist. The STRUCTURE analysis was also performed considering the two species separately (Figure 4B). A different situation can be observed for P. cupaniana and P. mahaleb. It is interesting to note that, while for P. mahaleb there is a division in K = 4 and the geographically distant populations show different gene pools, on the other hand the substructure of P. cupaniana is characterized by two gene pools. The MC is represented by a gene pool while the other three populations are grouped in another unique gene pool.

4. Discussion

To the best of our knowledge, this is the first in-depth study on the genetic diversity and structure of the Sicilian populations of Prunus mahaleb and the endemic Prunus cupaniana and the first to shed light on their probable different genetic identity. Our research contributes to providing information on the biodiversity of Sicilian species and can be considered a starting point for future programmes of conservation of local genetic resources. In the Mediterranean Basin, islands have been identified as one of the hotspots of plant diversity with 5500 plants, exhibiting an endemism rate of around 10% [38]. Among the large Mediterranean islands, Sicily hosts one of the richest and most diverse vascular floras, including 430 strictly endemic taxa [38]. Efforts to preserve biodiversity of this area and to maintain the species ability to survive in time of climate change must include the assessment and conservation of intraspecific genetic diversity. In this framework, our study follows the recommendations of IUCN (International Union for the Conservation of Nature) which emphasized the need to give greater consideration to genetic diversity when implementing projects aimed at the management and conservation of endangered plant species [39]. While recent studies have investigated the genetic diversity of P. mahaleb populations and accessions in Europe [10,40,41,42] and contributed to clarify the phylogenetic relationships between P. mahaleb and the Cherry species of agronomic interest [43,44], until now there are no reports on the genetic diversity and the genetic relationships of the Sicilian endemic P. cupaniana. Even if based on nine nuclear microsatellites markers our results of the PcoA and STRUCTURE analyses clearly show the genetic distinctness between P. mahaleb and P. cupaniana samples. The analysis conducted using STRUCTURE also highlights the complete absence of introgression between P. mahaleb and P. cupaniana even where they grow in close proximity, like in the case of Ficuzza and Rocca Busambra sites. Future more in-depth molecular analysis should be carried out to confirm these preliminary findings to support the taxonomic treatment of these two taxa as distinct species, as already reported by Pignatti [14], rather than relegating them to the subspecies or the variety rank, as previously proposed [22]. Their genetic isolation could be likely linked to a reproductive barrier (pollen and/or flower structure, flowering period, presence of specialized pollinators) that deserves to be further investigated. If confirmed at the rank of species, P. cupaniana should therefore be added to the already long list of woody species endemic to the Sicilian vascular flora [45,46].
Noteworthy are the high values of differentiation between populations of both P. mahaleb and P. cupaniana, which are not always observed in forest stands. The high values of Molecular Variance (AMOVA) and the high Fst are indications of very low or even absent intraspecific gene flow. Similar results were observed in other species with a scattered and localized distribution [47,48].
Gene flow among genetic clusters is probably low due to the small population size and the geographical and environmental setting of Sicilian sampling sites. Indeed, the investigated populations form small, isolated patches located at different altitudes and/or separated by strong physical barriers such as rocky cliffs that may represent an insurmountable obstacle for genetic exchanges between them.
This hypothesis is supported by findings from previous studies on P. mahaleb. For instance, Jordano and Godoy [8] observed that sharp elevation gradient induces a variation of 5–9 °C in mean weekly minimum temperature and 4 °C in mean maximum temperature during the reproductive period of the Spanish populations of P. mahaleb, causing a remarkable variation in the flowering and fruiting phenophases. Similar future research aimed at monitoring flowering times linked to temperatures and altitude gradients could provide more precise indications on the gene flow among Sicilian populations. A remarkably high number of clonal individuals was observed in all populations, especially in those belonging to P. cupaniana. This finding suggests the local prevalence of asexual reproduction through root suckers. This aspect should also be investigated further, taking into account that these species may be affected by the grazing pressure of herbivores on seedlings and young individuals.
Moreover, when small populations become spatially isolated, the magnitude of genetic variation decreases [49], while the percentage of private or rare alleles increases along with the divergence among populations [47]. The above findings support our results: high values of private allelic richness and a low genetic diversity was observed in all the P. mahaleb populations and in the MC and RB populations of P. cupaniana. In this context, our results also help to identify populations whose conservation is crucial for the in situ and ex situ preservation of both species. We suggest that the CA population of P. mahaleb and the RB population of P. cupaniana should be given priority for conservation. Indeed, these two populations showed the highest mean values of allelic richness and private allelic richness among all populations. To reduce the isolation of the investigated populations and to re-establish the gene flow among them, consideration should be given to the possibility of creating intermediate populations that ensure greater ecological connectivity, which in turn would greatly contribute to increase the values of heterozygosity and allelic richness. Moreover, to enhance and conserve the Sicilian germplasm of P. mahaleb, genetic data from its insular populations should be compared with findings from other Italian regions and other European countries. Such investigations would shed light on the natural history of the species and clarify whether its migration path was only mediated by frugivorous animals, or whether it also reflects deliberate human introductions. Indeed, as has been suggested for numerous other woody species of agronomic interest (e.g., vine, olive, chestnut, walnut, hazelnut, pear, pomegranate, stone pine, carob), the role played by introductions made at different times by the peoples who have ruled the island during the last 3000 years, namely the Phoenicians, Greeks and Romans, the Byzantines and Arabs, and the French and Spanish, cannot be underestimated.

5. Conclusions

The results presented here provide an overview of the genetic structure of the Sicilian populations of two woody Rosaceae that are uncommon in Sicily, Prunus mahaleb and Prunus cupaniana. Although some limitations should be acknowledged, including the number and nature of the microsatellite markers used, the limited number of individuals analyzed and the high percentage of clonal individuals observed, our results indicated a clear genetic differentiation between P. mahaleb and P. cupaniana. Moreover, if future genome-based studies validate the recognition of P. cupaniana at the species rank, it should be included among the endemic woody flora of Sicily.
The data obtained from this study may be used to guide future forest management strategies and inform actions aimed at maintaining genetic diversity.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/d18070438/s1, Figure S1: Distribution range of P. mahaleb and P. cupaniana; Table S1: clonal individuals; Table S2: Raw data matrix.

Author Contributions

Conceptualization, C.M., T.L.M. and S.P.; methodology, C.M., S.P. and T.L.M.; software, C.M.; validation, C.M. and S.P.; laboratory analysis, M.C. and L.L.; sampling, G.C., G.T., L.L. and M.C.; data curation, C.M.; writing—original draft preparation, C.M. and S.P.; writing—review and editing, T.L.M., E.B. and S.P.; funding acquisition, T.L.M. All authors have read and agreed to the published version of the manuscript.

Funding

This study was carried out within the project “Studio per l’implementazione delle specie per le quali è obbligatoria la raccolta di materiale di moltiplicazione”, funded by Dipartimento Regionale dello Sviluppo Rurale e Territoriale-Assessorato Regionale dell’Agricoltura, dello Sviluppo Rurale e della Pesca Mediterranea—Regione Siciliana, in the framework of the Rural Development Programme (PSR) “Sicilia 2014–2020, Sottomisura 15.2” Assessorato Regionale dell’Agricoltura, dello Sviluppo Rurale e della Pesca Mediterranea—Regione Siciliana, nell’ambito del PSR Sicilia 2014–2020, Sottomisura 15.2.

Data Availability Statement

The raw microsatellite data are available in the Supplementary Material Table S2.

Acknowledgments

The authors thanks for their valuable support, A. Sidoti, head of the territorial agency of Catania of the Dipartimento Sviluppo Rurale e Territoriale DSRT and A. C. Grasso head of the unit for territorial valorisation and management of the province agency of Catania of DSRT. The authors also thanking several friends and colleagues for helping with the sampling activities: Giovanni Giardina (Rocca Busambra-Ficuzza), Alessandro Crisafulli, Francesco Anania, Riccardo Guarino and Noa Terracina (Peloritani Mts.).

Conflicts of Interest

The authors declare no conflict of interest.

References

  1. Gapare, W.J. Merging applied gene conservation activities with advanced generation breeding initiatives: A case study of Pinus radiata D. Don. New For. 2014, 45, 311–331. [Google Scholar]
  2. Reed, D.H.; Frankham, R. Correlation between fitness and genetic diversity. Conserv. Biol. 2003, 17, 230–237. [Google Scholar] [CrossRef] [Scilit]
  3. Suoto, C.P.; Mathiasen, P.; Acosta, M.C.; Quiroga, M.P.; Vidal-Russell, R.; Echeverria, C.; Premoli, A.C. Identifying genetic hotspots by mapping molecular diversity of widespread trees: When commonness matters. J. Hered. 2015, 6, 537–545. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Fussi, B.; Seho, M.; Kavaliauskas, D. In situ and ex situ conservation measures. In Ecological Connectivity of Forest Ecosystems; Lapin, K., Oettel, J., Braun, M., Konrad, H., Eds.; Springer: Cham, Switzerland, 2025. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Volis, S.; Blecher, M. Quasi in situ: A bridge between ex situ and in situ conservation of plants. Biodivers. Conserv. 2010, 19, 2441–2454. [Google Scholar] [CrossRef] [Scilit]
  6. Pasta, S.; La Mantia, T.; Clementi, G.; Traina, G.; Cherubini, M.; Leonardi, L.; Mattioni, C. Le indagini genetiche sulle specie forestali siciliane. In I Boschi di Sicilia tra Strategie di Conservazione e di Ampliamento; Pasta, S., La Mantia, T., Eds.; Publisher Danaus: Palermo, Italy, 2025; Volume 1, Cap III, pp. 73–101. ISBN 978-88-97603-54-2. [Google Scholar]
  7. Webb, D.A. Prunus L. In Flora Europaea. Volume 2. Rosaceae to Umbelliferae; Tutin, T.G., Heywood, V.H., Burges, N.A., Valentine, D.H., Walters, S.M., Webb, D.A., Eds.; Cambridge University Press: Cambridge, UK, 1968; pp. 77–80. [Google Scholar]
  8. Jordano, P.; Godoy, J.A. RAPD variation and population genetic structure in Prunus mahaleb (Rosaceae), an animal-dispersed tree. Mol. Ecol. 2000, 9, 1293–1305. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Ozyurt, I.K.; Akca, Y.; Ercisli, S. Molecular charaxcterization of Prunus mahaleb L. rootstock candidates by ISSR markers. Genetika 2013, 45, 717–726. [Google Scholar] [CrossRef] [Scilit]
  10. Abedian, M.; Talebi, M.; Sayed-Tabatabaei, B.E.; Ghobadi, C. Chloroplast microsatellite diversity among and within Prunus mahaleb L. and P. avium L. species. J. Agric. Sci. 2012, 4, 191–202. [Google Scholar] [CrossRef] [Scilit]
  11. Barth, D. Prunus mahaleb . In Enzyklopädie der Holzgewächse: Handbuch und Atlas der Dendrologie; Roloff, A., Weisgerber, H., Lang, U., Stimm, B., Schutt, P., Eds.; Wiley-VCH Verlag: Weinheim, Germany, 1996; Volume 3. [Google Scholar]
  12. Browicz, K. Chorology of Trees and Shrubs in South-West Asia and Adjacent Regions; Bogucki Wydawnictwo Naukowe: Poznań, Poland, 1996; p. 48. [Google Scholar]
  13. Charco, J. Guía a los Arboles y Arbustos del Norte de África; Clave de Determinación, Descripciones, Ilustraciones y Mápas de Distribución; Agencia Española de Cooperación Internacional: Madrid, Spain, 2001; 671p. [Google Scholar]
  14. Pignatti, S. Prunus L. In Flora d’Italia, 2nd ed.; Pignatti, S., Guarino, R., La Rosa, M., Eds.; Bologna-Edagricole New Business Media: Bologna, Italy; Milano, Italy, 2017; Volume 2, pp. 819–827. [Google Scholar]
  15. Pasta, S.; Badalamenti, E.; Clementi, G.; La Mantia, T.; Traina, G. Cap. II—Specie per la quali non esistevano siti di raccolta. In I Boschi di Sicilia tra Strategie di Conservazione e di Ampliamento; La Mantia, T., Badalamenti, E., Clementi, G., Pasta, S., Tranina, G., Eds.; Publisher Danaus: Palermo, Italy, 2025; Volume 1, Cap. III; pp. 35–95. ISBN 978-88-97603-56-6. [Google Scholar]
  16. Raimondo, F.M.; Spadaro, V. Nomenclatural and taxonomic remarks on Prunus cupaniana (Rosaceae) from Sicily. Bocconea 2012, 24, 5–12. [Google Scholar]
  17. Gussone, G. Prunus . In Supplementum ad Florae Siculae Prodromum, Quod et Specimen Florae Insularum Siciliae Ulteriori Adjacentium; Ex Regia Typographia: Neapoli, Italy, 1832; Volume 1, pp. 562–564. [Google Scholar]
  18. Gussone, G. Prunus . In Florae Siculae Synopsis Exhibens Plantas Vasculares in Sicilia Insulisque Adjacentibus Hucusque Detectas Secundum Systema Linneanum Dispositas; Typ. Tramater: Neapoli, Italy, 1843; Volume 1, pp. 552–553. [Google Scholar]
  19. Arcangeli, G. Prunus L. In Compendio della Flora Italiana Ossia Manuale per la Determinazione delle Piante che Trovansi Selvatiche od Inselvatichite Nell’italia o Nelle Isole Adiacenti; E. Leoscher: Torino, Italy, 1882; pp. 209–211. [Google Scholar]
  20. Pénzes, A. Új Prunus-változatok. I. (Neue Prunus-Varietäten. I.).[=New varieties of Prunus]. Bot. Közlem. 1958, 47, 287–295. [Google Scholar]
  21. Soják, J. Problematics in the classification and categorization of Mahaleb cherries. Časopis Národního Muz. Praze Rada Přír. 1985, 153, 171. [Google Scholar]
  22. Bartolucci, F.; Peruzzi, L.; Galasso, G.; Alessandrini, A.; Ardenghi, N.M.G.; Bacchetta, G.; Banfi, E.; Barberis, G.; Bernardo, L.; Bouvet, D.; et al. A second update to the checklist of the vascular flora native to Italy. Plant Biosyst. 2024, 158, 219–296. [Google Scholar] [CrossRef] [Scilit]
  23. Nyman, C.F. Prunus L. In Conspectus Floræ Europæ (Ranunculaceæ-Pomaceæ); Typis Officinæ Bohlinianæ: Örebro, Sweeden, 1878; pp. 212–214. [Google Scholar]
  24. Lojacono-Pojero, M. Prunus Lin. In Flora Sicula o Descrizione delle Piante Spontanee o Indigenate in Sicilia, (Polypetalae-Calyciflorae); Tipografia dello Statuto: Palermo, Italy, 1891; Volume 1, pp. 163–164. [Google Scholar]
  25. Fiori, A. Prunus mahaleb . In Flora Analitica d’Italia, Ossia Descrizione delle Piante Vascolari Indigene Inselvatichite e Largamente Coltivate in Italia Disposte per Quadri Analitici; Fiori, A., Paoletti, G., Eds.; Tip. del Seminario: Padova, Italy, 1898; Volume 1, p. 561. [Google Scholar]
  26. Fiori, A. Prunus mahaleb . In Nuova Flora Analitica d’Italia. Contenente la Descrizione delle Piante Vasco/Ari Indigene Inselvatichite e Largamente Coltivate in Italia; Tip. M. Ricci: Firenze, Italy, 1924; Volume 1, p. 735. [Google Scholar]
  27. Ascherson, P.F.A.; Graebner, K. Band 6(2) Abtheilung [Rosaceae (Pomoideae, Prunoideae); Leguminosae]. In Synopsis der Mitteleuropäischen Flora; Wilhelm Engelmann: Leipzig, Germany, 1906; pp. 136–165. [Google Scholar]
  28. Cupani, F. Panphyton Siculum; Ex Typographia regia A. Epiro: Panormi, Italy, 1713; Volume 3. [Google Scholar]
  29. Camerano, P.; Cullotta, S.; Varese, P. (Eds.) Strumenti Conoscitivi per la Gestione delle Risorse Forestali della Sicilia. Tipi Forestali; Compagnia delle Foreste: Arezzo, Italy; Regione Siciliana: Palermo, Italy, 2011; p. 91. [Google Scholar]
  30. Vaughan, S.P.; Russell, K. Characterization of novel microsatellites and development of multiplex PCR for large-scale population studies in wild cherry, Prunus avium. Mol. Ecol. Notes 2004, 4, 429–431. [Google Scholar] [CrossRef] [Scilit]
  31. Testolin, R.; Marrazzo, T.; Cipriani, G.; Quarta, R.; Verde, I.; Dettori, M.T.; Pancaldi, M.; Sansavini, S. Microsatellite DNA in peach Prunus persica (L.) Batsch and its use in fingerprinting and testing the genetic origin of cultivars. Genome 2000, 43, 512–520. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Downey, S.L.; Iezzoni, A.F. Polymorphic DNA markers in black cherry (Prunus serotina) are identified using sequences from sweet cherry peach, and sour cherry. J. Am. Soc. Hortic. Sci. 2000, 125, 76–80. [Google Scholar] [CrossRef] [Scilit]
  33. Peakall, R.; Smouse, P.E. GenAlEX 6.5: Genetic analysis in Excel. Population genetic software for teaching and research: An update. Bioinformatics 2012, 28, 2537–2539. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Kalinowski, S.T. HP-Rare: A computer program for performoring rarefaction on measures of allelic diversity. Mol. Ecol. Notes 2005, 5, 187–189. [Google Scholar] [CrossRef] [Scilit]
  35. Pritchard, J.K.; Stephens, M.; Donnelly, P. Inference of population structure using multilocus genotype data. Genetics 2000, 155, 945–959. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Evanno, G.; Regnaut, S.; Goudet, J. Detecting the number of clusters of individuals using the software Structure: A simulation study. Mol. Ecol. 2005, 14, 2611–2620. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Earl, D.A.; vonHoldt, B.M. Structure Harvester: A website and program for visualizing Structure output and implementing the Evanno method. Conserv. Genet. Resour. 2012, 4, 359–361. [Google Scholar]
  38. Pasta, S.; Médail, F.; Panitsa, M. The vascular flora and the plant communities of the Mediterranean Islands: A biogeographical and historical sketch. In Herpetofauna of the Islands of the Mediterranean Basin; Corti, C., Leviton, A., Lo Cascio, P., Sindaco, R., Eds.; Danaus: Palermo, Italy, 2026; pp. 1–61. [Google Scholar]
  39. Scotti-Saintagne, C.; de Sousa Rodrigues, A.; Roig, A.; Fady, B. A comprehensive strategy for the conservation of forest tree genetic diversity: An example with the protected Pinus nigra subsp. salzmannii (Dunal) Franco in France. Conserv. Genet. 2024, 25, 469–480. [Google Scholar]
  40. Barac, D.; Ognjanov, V.; Obreht, D.; Ljubojevic, M.; Bosnjakovic, D.; Pejic, I.; Gasic, K. Genotypic and phenotypic diversity of cherry species collected in Serbia. Plant Mol. Biol. Rep. 2014, 32, 92–108. [Google Scholar] [CrossRef] [Scilit]
  41. Turkoglu, Z.; Bilgener, S.; Ercisli, S.; Yildirim, N. Simple sequence repeat (SSR) analysis for assessment of genetic variability in wild cherry germplasm. J. Appl. Bot. Food Qual. 2012, 85, 229–233. [Google Scholar]
  42. Abedian, M.; Talebi, M.; Golmohammdi, H.R.; Sayed-Tabatabaei, B.H. Genetic diversity and population structure of mahaleb cherry (Prunus mahaleb L.) and sweet cherry (Prunus avium L.) using SRAP markers. Biochem. Syst. Ecol. 2012, 40, 112–117. [Google Scholar] [CrossRef] [Scilit]
  43. Song, Y.F.; Zhang, C.; Idrees, M.; Yi, X.; Wang, X.R.; Li, M. Molecular phylogenetics and biogeography reveal the origin of cherries (Prunus subg. Cerasus, Rosaceae). Bot. J. Linn. Soc. 2024, 204, 304–315. [Google Scholar] [CrossRef] [Scilit]
  44. Shen, X.; Li, Y.; Jiang, D.; Liu, Y. Creating an effective DNA identification system for discriminating cherries (Prunus subgenus Cerasus). BMC Plant Biol. 2025, 25, 475. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Raimondo, F.M. Biodiversità nella dendroflora italiana. L’Italia For. Mont. 2013, 5, 233–257. [Google Scholar] [CrossRef] [Scilit]
  46. Brullo, C.; Brullo, S. Flora Endemica Illustrata della Sicilia; Laruffa (Ed): Reggio Calabria, Italy, 2020; p. 441. [Google Scholar]
  47. Stevanoski, I.; Lakušić, D.; Kuzmanović, N.; Mitić, D.; Glasnović, P.; Shuka, D.; Radosavljević, I. Ecological and genetic differentiation decoupled in an endemic species, Campanula hawkinsiana (Campanulaceae). Bot. J. Linn. Soc. 2006, boag009. [Google Scholar] [CrossRef] [Scilit]
  48. Vandepitte, K.; Gristina, A.S.; De Raedt, R.; Roldan-Ruiz Marcenò, C.; Sciandrello, S.; Honnay, O. Conservation genetics of endemics from Mediterranean Basin: High genetic differentiation but no genetic diversity loss from the last populations of grape Hyacinth Leopoldia gussonei. Conserv. Genet. 2013, 14, 963–972. [Google Scholar] [CrossRef] [Scilit]
  49. Morgan, J.W.; Meyer, M.J.; Young, A.G. Severe habitat fragmentation leads to declines in genetic variation, mate availability and reproductive success in small populations of a once-common Australian grassland Daisy. Int. J. Plant Sci. 2013, 174, 1209–1218. [Google Scholar] [CrossRef] [Scilit]
Figure 1. (A) Prunus mahaleb, detail of leaves and fruits; (B) Prunus cupaniana, detail of leaves and flowers; (C) the stand of P. cupaniana located on the screen slopes of Serra di Quacella (QU) shows clear signs of over browsing by fallow deers; (D) the P. mahaleb stand at Alcara Li Fusi (AL) is characterized by a high amount of rock outcrops.
Diversity 18 00438 g001
Figure 2. Sampling sites P. cupaniana (blue dots) and P. mahaleb (red dots).
Diversity 18 00438 g002
Figure 3. Principal Coordinate Analysis (PCoA) (A) based on pair-wise genetic distance on the complete set of individuals; (B) based on the Fst among populations. (A) each population is represented with a different colour; P. mahaleb populations = AL, CA, ER, PV; P. cupaniana populations MC, NE, QU, RB.
Diversity 18 00438 g003
Figure 4. Population structure inferred for the 93 samples of P. mahaleb and P. cupaniana by Bayesian assignment using STRUCTURE software, different colours indicated the individual’s membership, populations are separated by a vertical black line; (A) K = 2 genetic distinctness of the two taxa (B) populations structure considering P. mahaleb and P. cupaniana separately.
Diversity 18 00438 g004
Table 1. Identity code (ID), sampling location, geographical and ecological characteristics, habit and threats of the 8 populations of P. mahaleb and P. cupaniana.
Pop IDSite Nb. of Samples LatLongAltitude (m a.s.l.)HabitatVegetative StatusGrowth HabitThreats
QUQuacella (Madonie)1537.85756014.0239691550–1620Scree and shrubland nucleiVery goodShrubGrazing
P. cupaniaMCMonte Cervi (Madonie)1837.87576913.9840921550–1600Scree and forest edges GoodProstrate shrubGrazing
RBRocca Busambra (Sicani)1537.85557513.4081311425–1475Shrubland nucleiVery goodShrubGrazing
NENeviere (Ficuzza Sicani)1637.85832413.3886011075–1145Scree and forest edgesGoodProstrate shrubRock collapse
Total 64
ERErice (Trapani)1438.03685612.594021650–750Forest nuclei on screeVery goodTree and shrubFire
P. mahalebPVPortella del Vento (Ficuzza Sicani)2037.84570313.4364261050–1100Forest nuclei on screeVery goodTreeGrazing
ALAlcara Li Fusi (Nebrodi Mts.)1538.00447314.726213650–700Forest nuclei on screeVery goodTreeGrazing
CACastroreale (Peloritani Mts.)538.08358915.232069750–780Forest edgesVery goodTreen.a.
Total 54
Table 2. Genetic diversity of the 93 sampled individuals of P. cupaniana and P. mahaleb. N = number of individuals; Ne = effective number of alleles per locus; I = Shannon genetic diversity index; Ho = observed, He = expected and uHe = unbiased heterozygosity; Fis = inbreeding coefficient.
NNeIHoHeuHeFis
P. cupanianaMean412.710.9640.2440.4790.4850.438
SE 0.640.220.0640.0890.0910.126
P. mahalebMean524.1751.6320.5240.7350.7420.28
SE 0.510.1040.040.0290.030.054
Table 3. Genetic diversity of the 8 surveyed Prunus populations. N = number of individuals; Ne = effective number of alleles per locus; I = Shannon genetic diversity index; Ho = observed, He = expected and uHe = unbiased heterozygosity; Ar = allelic richness; PAr = private allelic richness; Fis = inbreeding coefficient; and Fst = diversity among populations.
Pop IDNNeIHoHeuHeArPArFisFst
MC182.1510.6940.330.3750.3852.440.550.07
P. cupanianaNE61.3130.1840.0220.110.111.2900.444
QU41.2520.1780.1670.1110.1271.310.13−0.047
RB132.2700.7170.2480.370.3852.590.730.272
All pops 0.376
AL152.2390.9030.5160.5110.5282.820.59−0.049
P. mahalebCA53.0181.1880.7330.6130.6814.332.58−0.197
ER131.4810.4350.3590.2750.2861.770.15−0.229
PV193.0631.1310.5910.5840.6003.651.02−0.028
All pops 0.361
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.