

Methicillin-Resistant Staphylococcus aureus in the Food Chain: Molecular Epidemiology, Resistance Mechanisms, and Public Health Implications

Abstract
1. Introduction
2. Literature Search Strategy
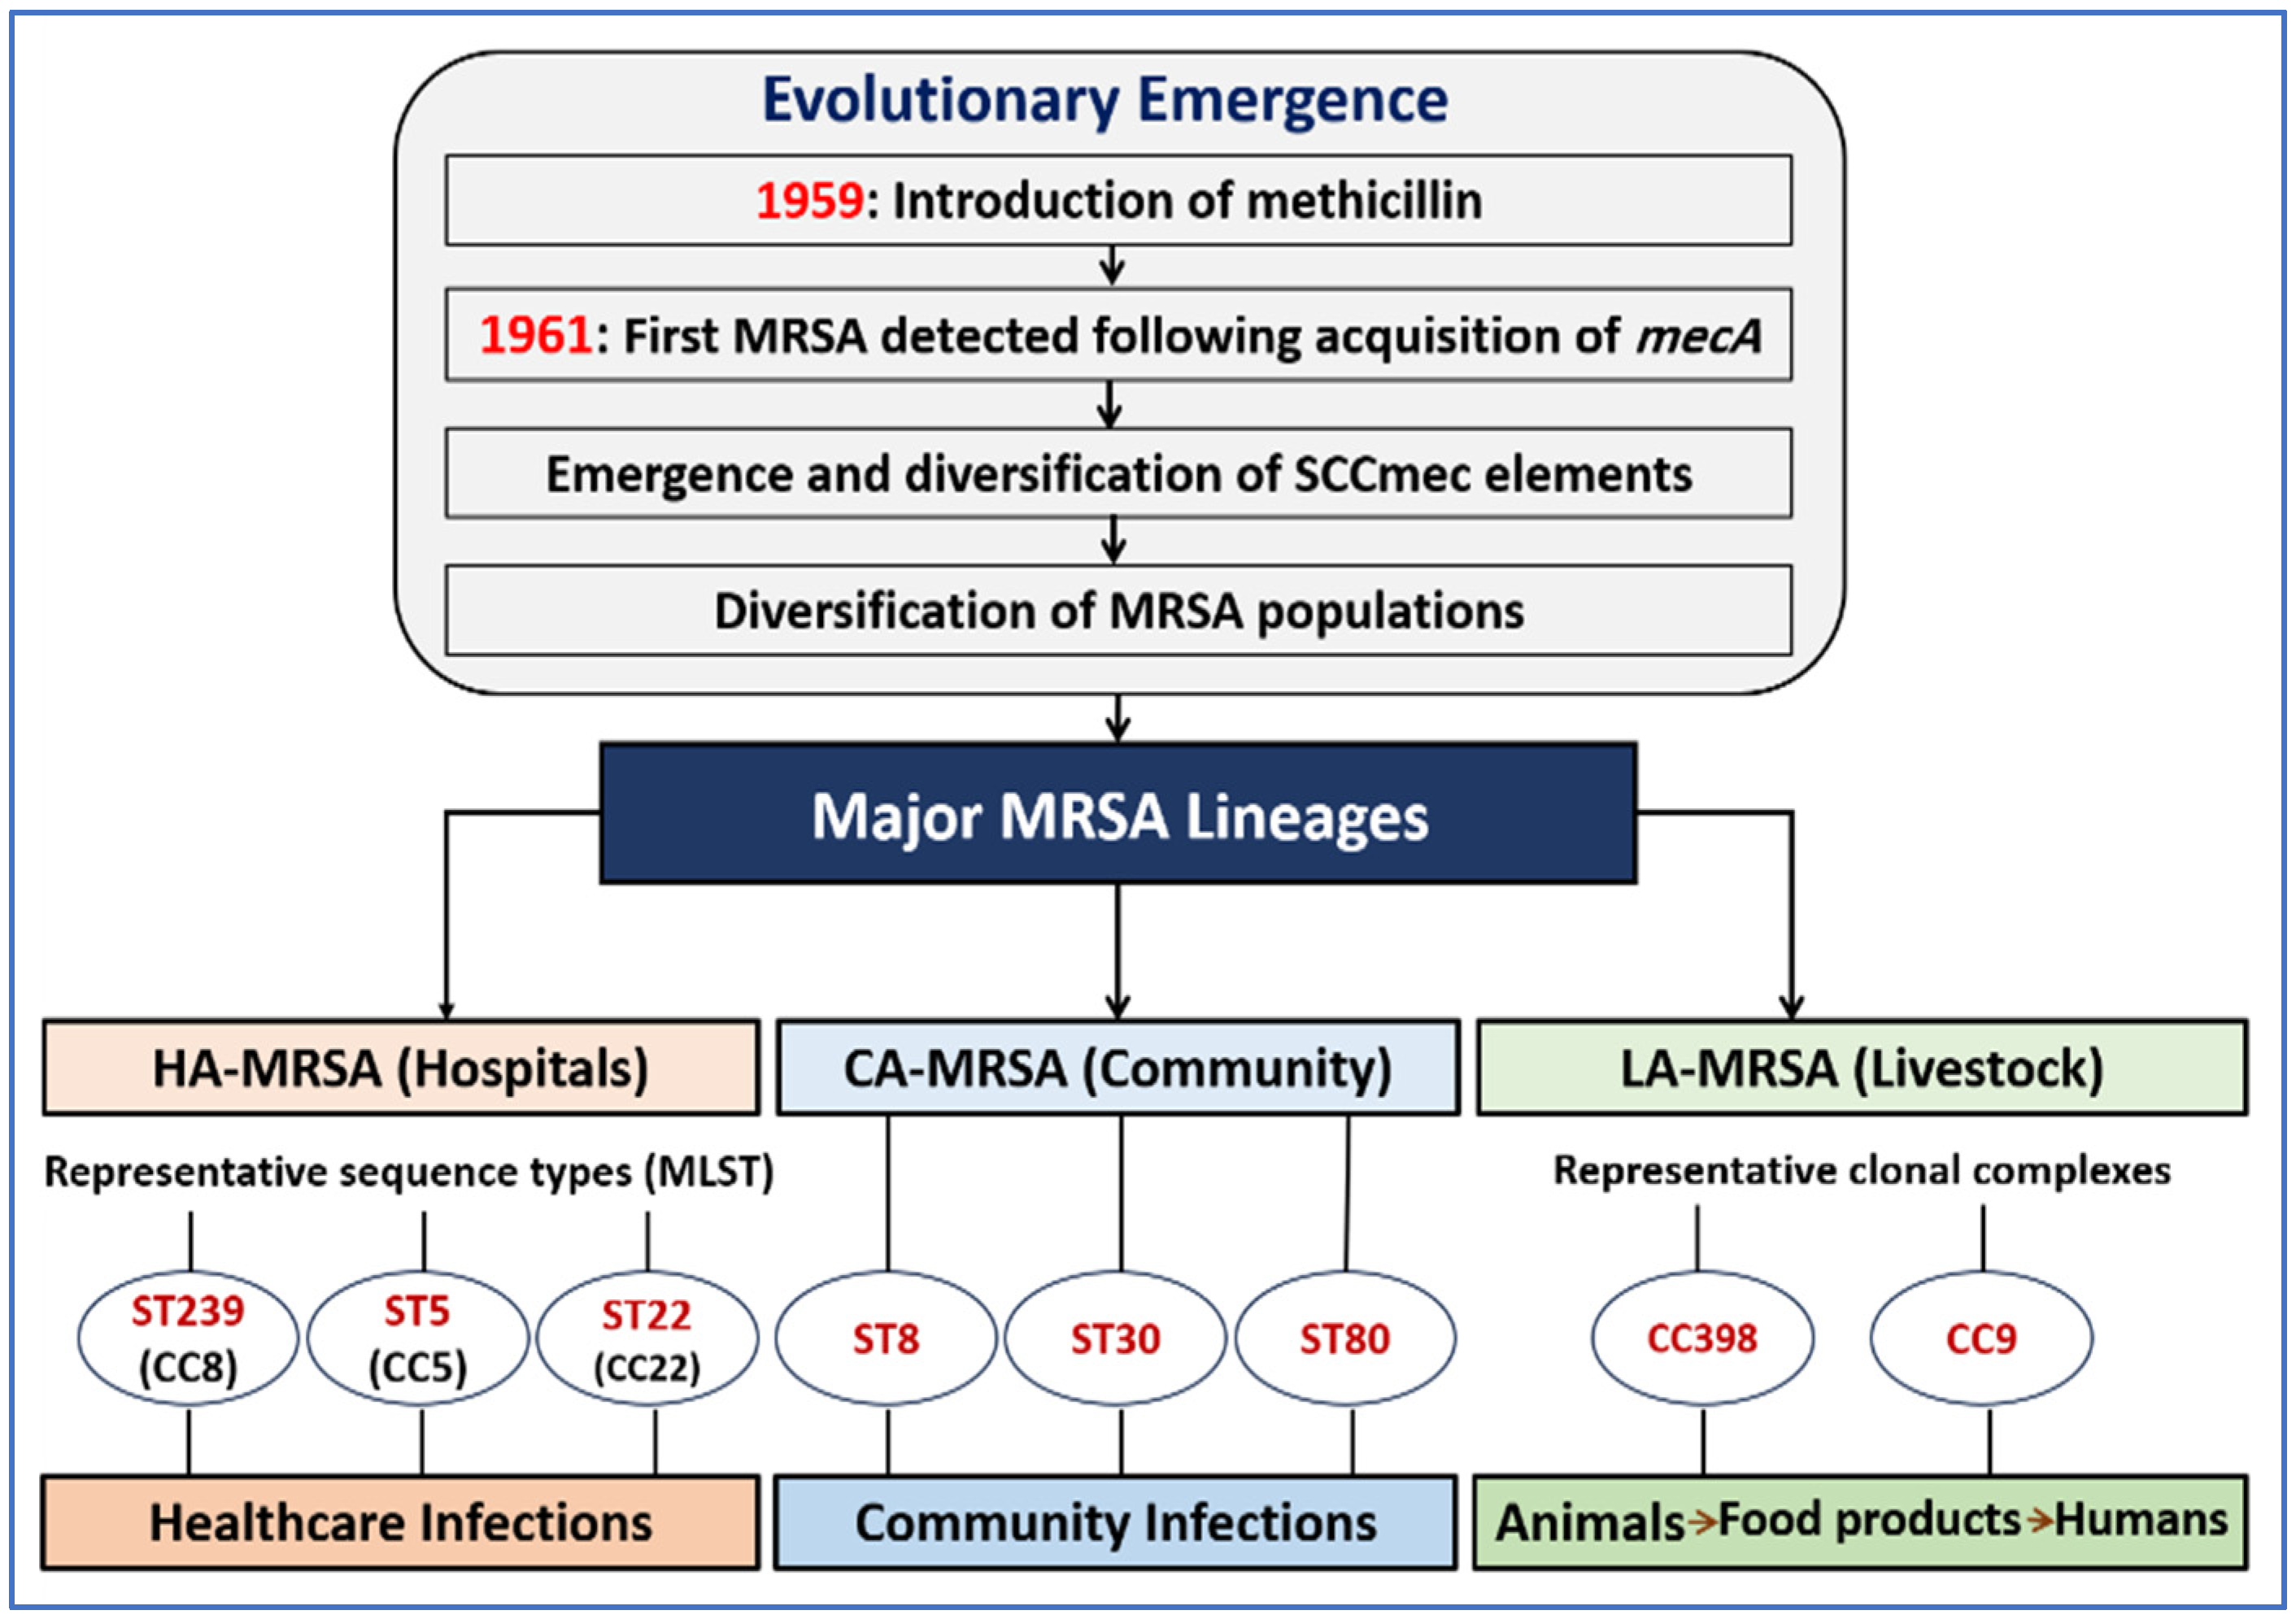
3. Evolutionary Emergence and Epidemiological Lineages of MRSA
3.1. Emergence of Methicillin Resistance in S. aureus
3.2. Major Epidemiological Lineages of MRSA
3.3. Adaptation of MRSA to Livestock Reservoirs
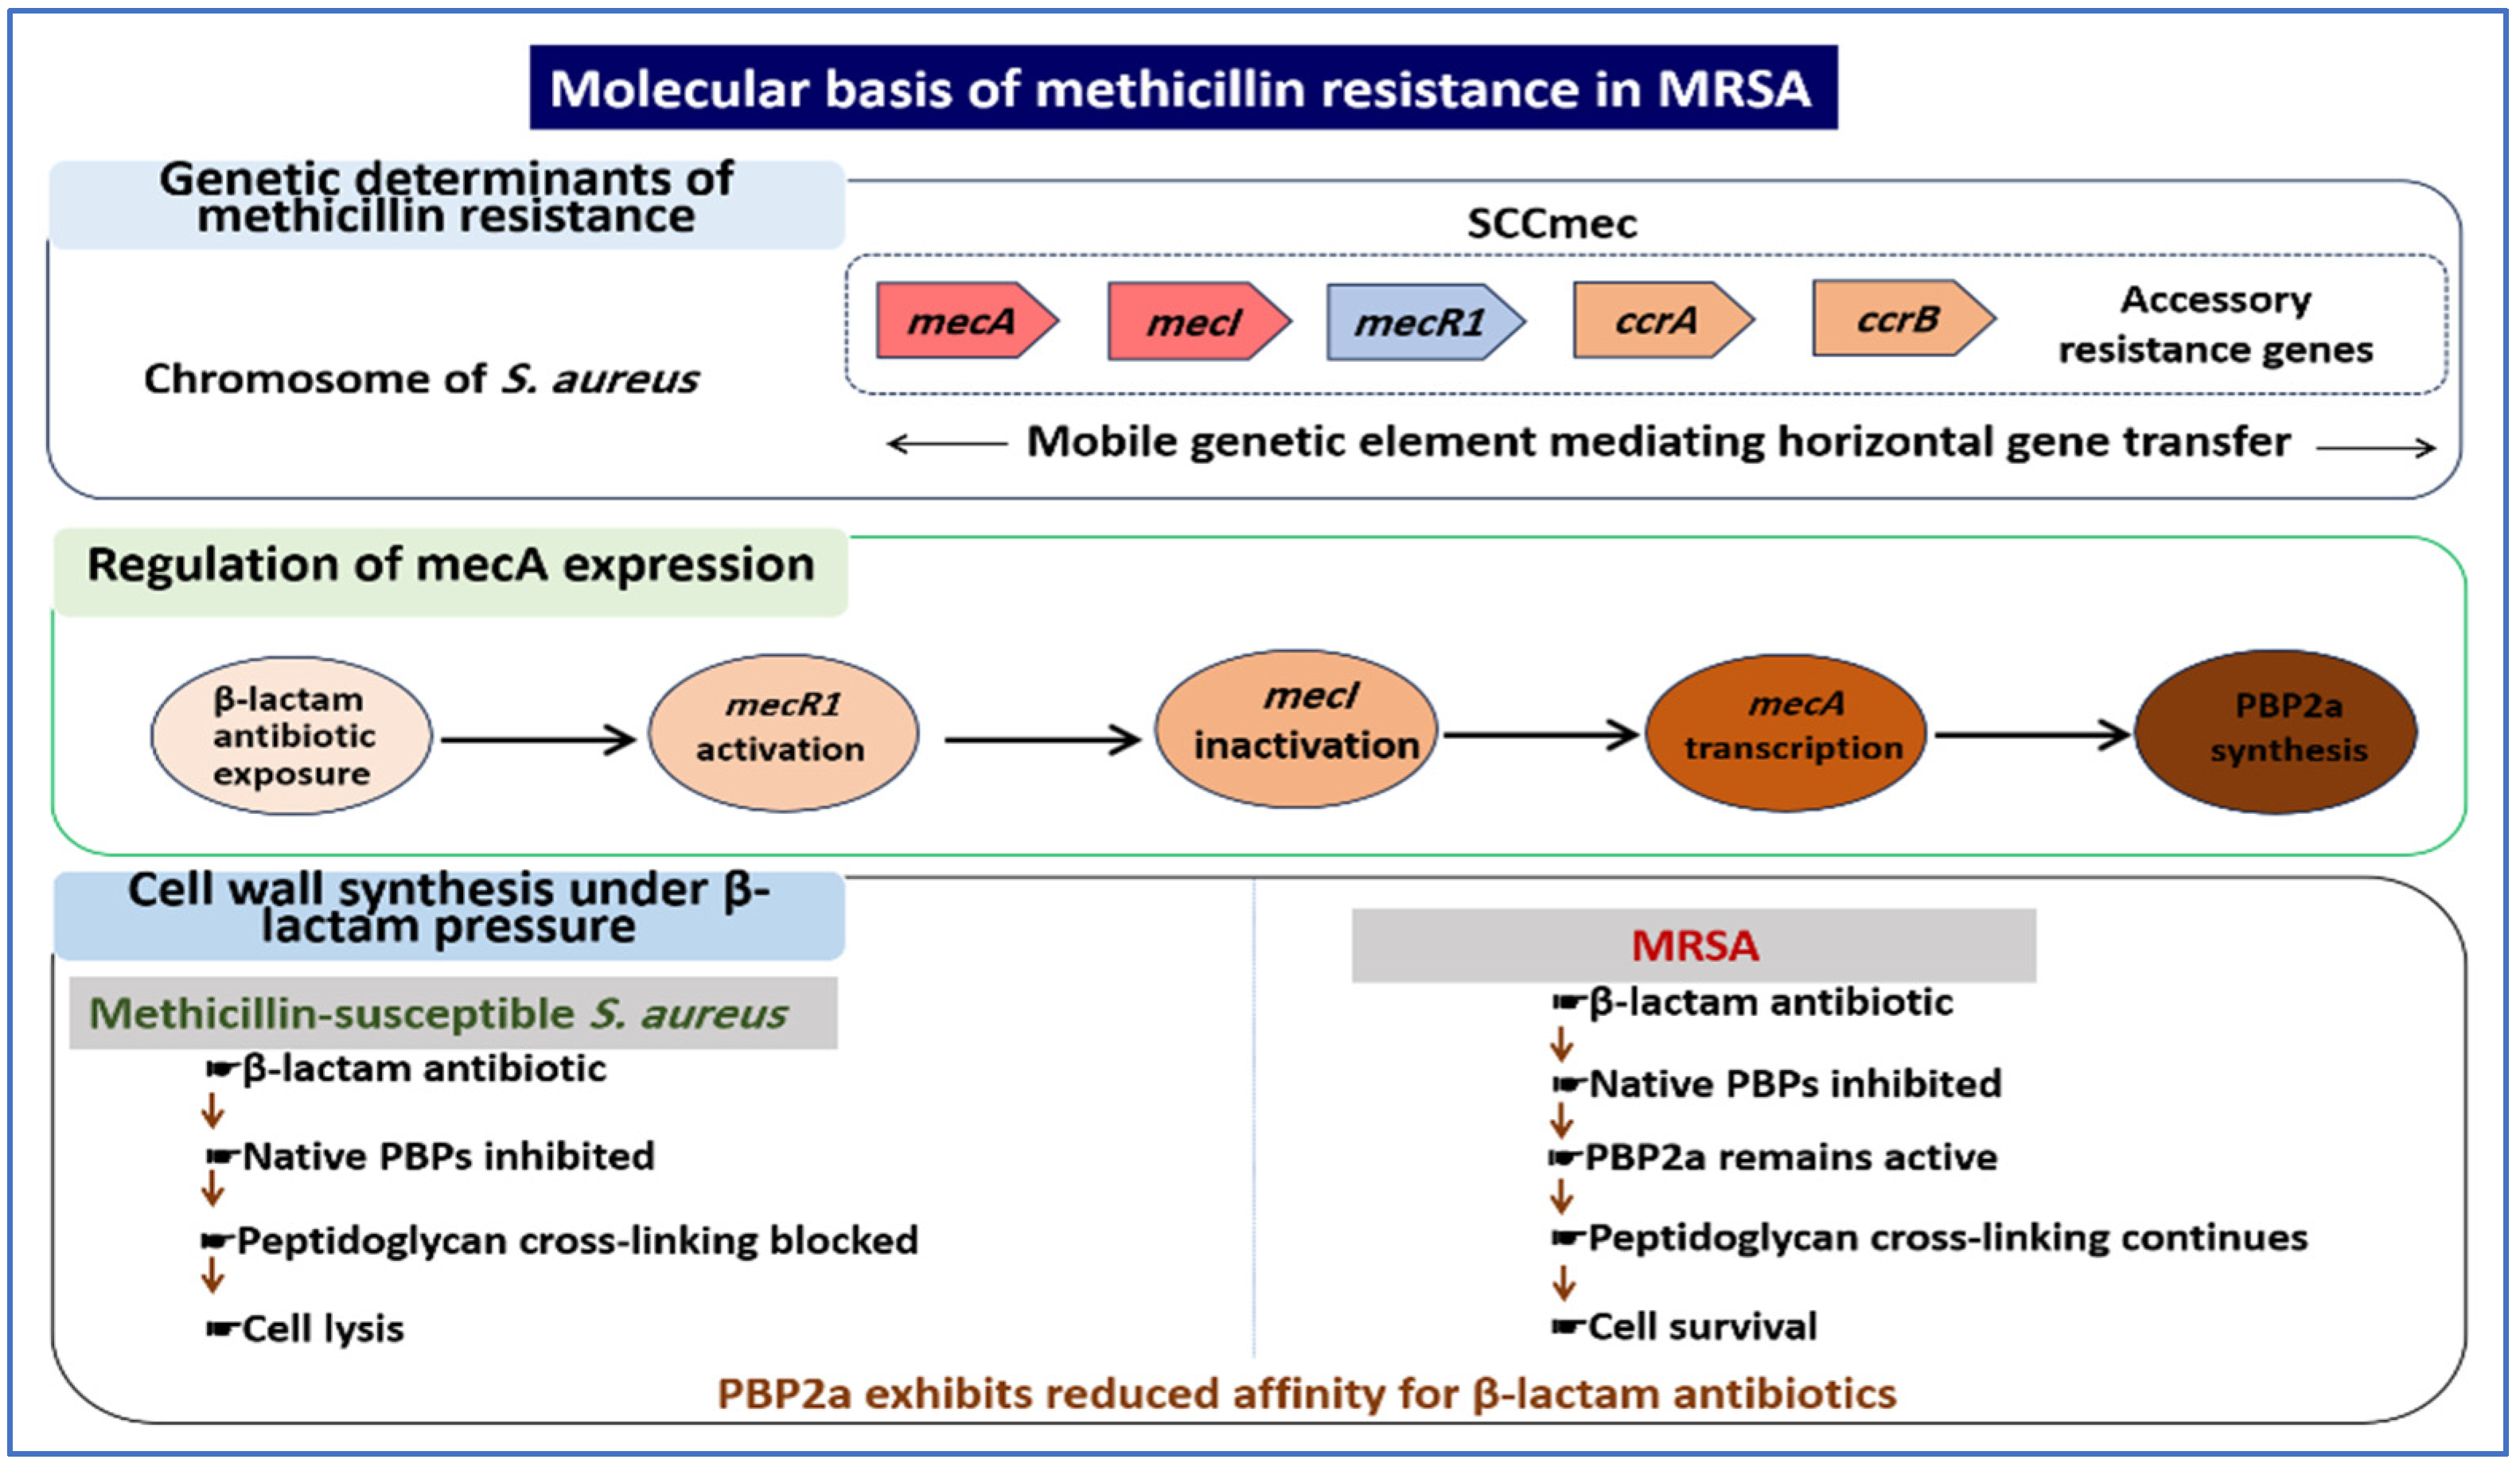
4. Molecular Basis of Methicillin Resistance
4.1. The mec Gene Complex
4.2. Structure and Function of PBP2a
4.3. Staphylococcal Cassette Chromosome mec (SCCmec)
4.4. Auxiliary Resistance Factors
4.5. Evolution of SCCmec Elements
5. Multidrug Resistance Determinants in MRSA
5.1. Macrolides and Lincosamides
5.2. Tetracycline
5.3. Fluoroquinolone
5.4. Efflux Systems and Environmental Selection
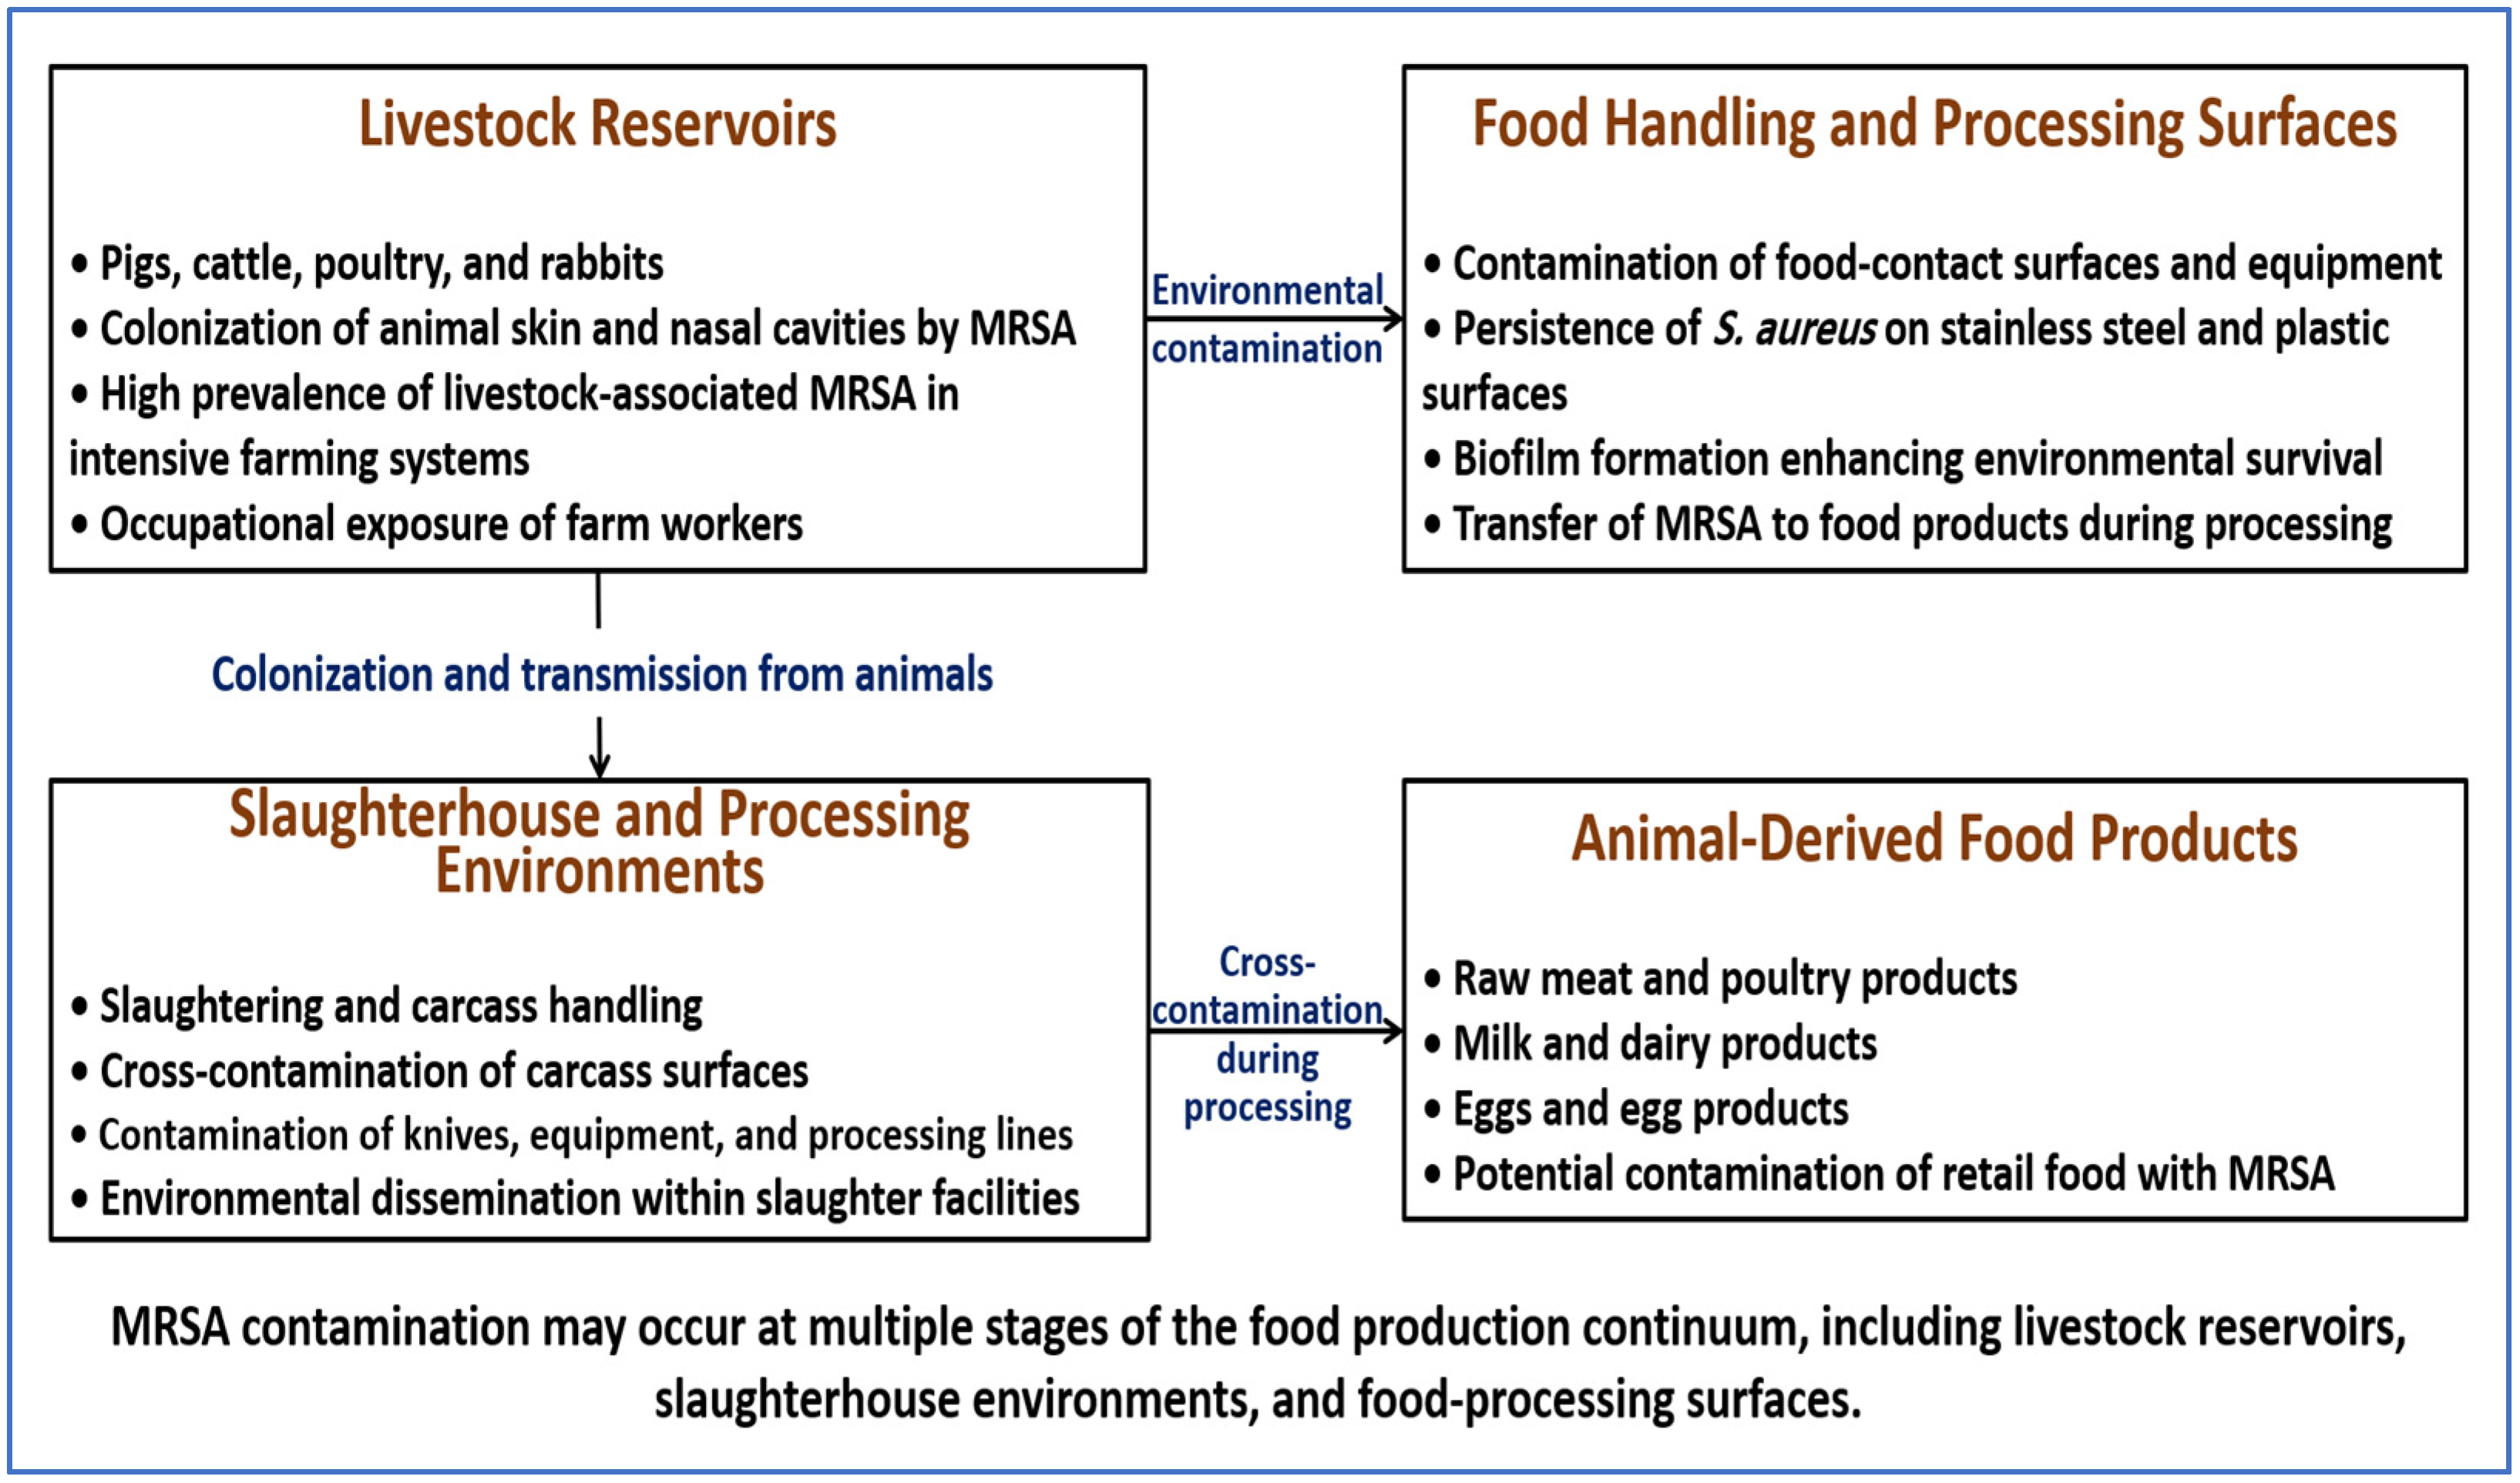
6. MRSA Reservoirs in the Food Production Continuum
6.1. Livestock Reservoirs
6.2. Slaughterhouse and Processing Environments
6.3. Food Handling and Processing Surfaces
7. Occurrence of MRSA in Food Products
7.1. Raw Animal-Derived Food Products
7.2. RTE Foods
7.3. Global Distribution and Prevalence
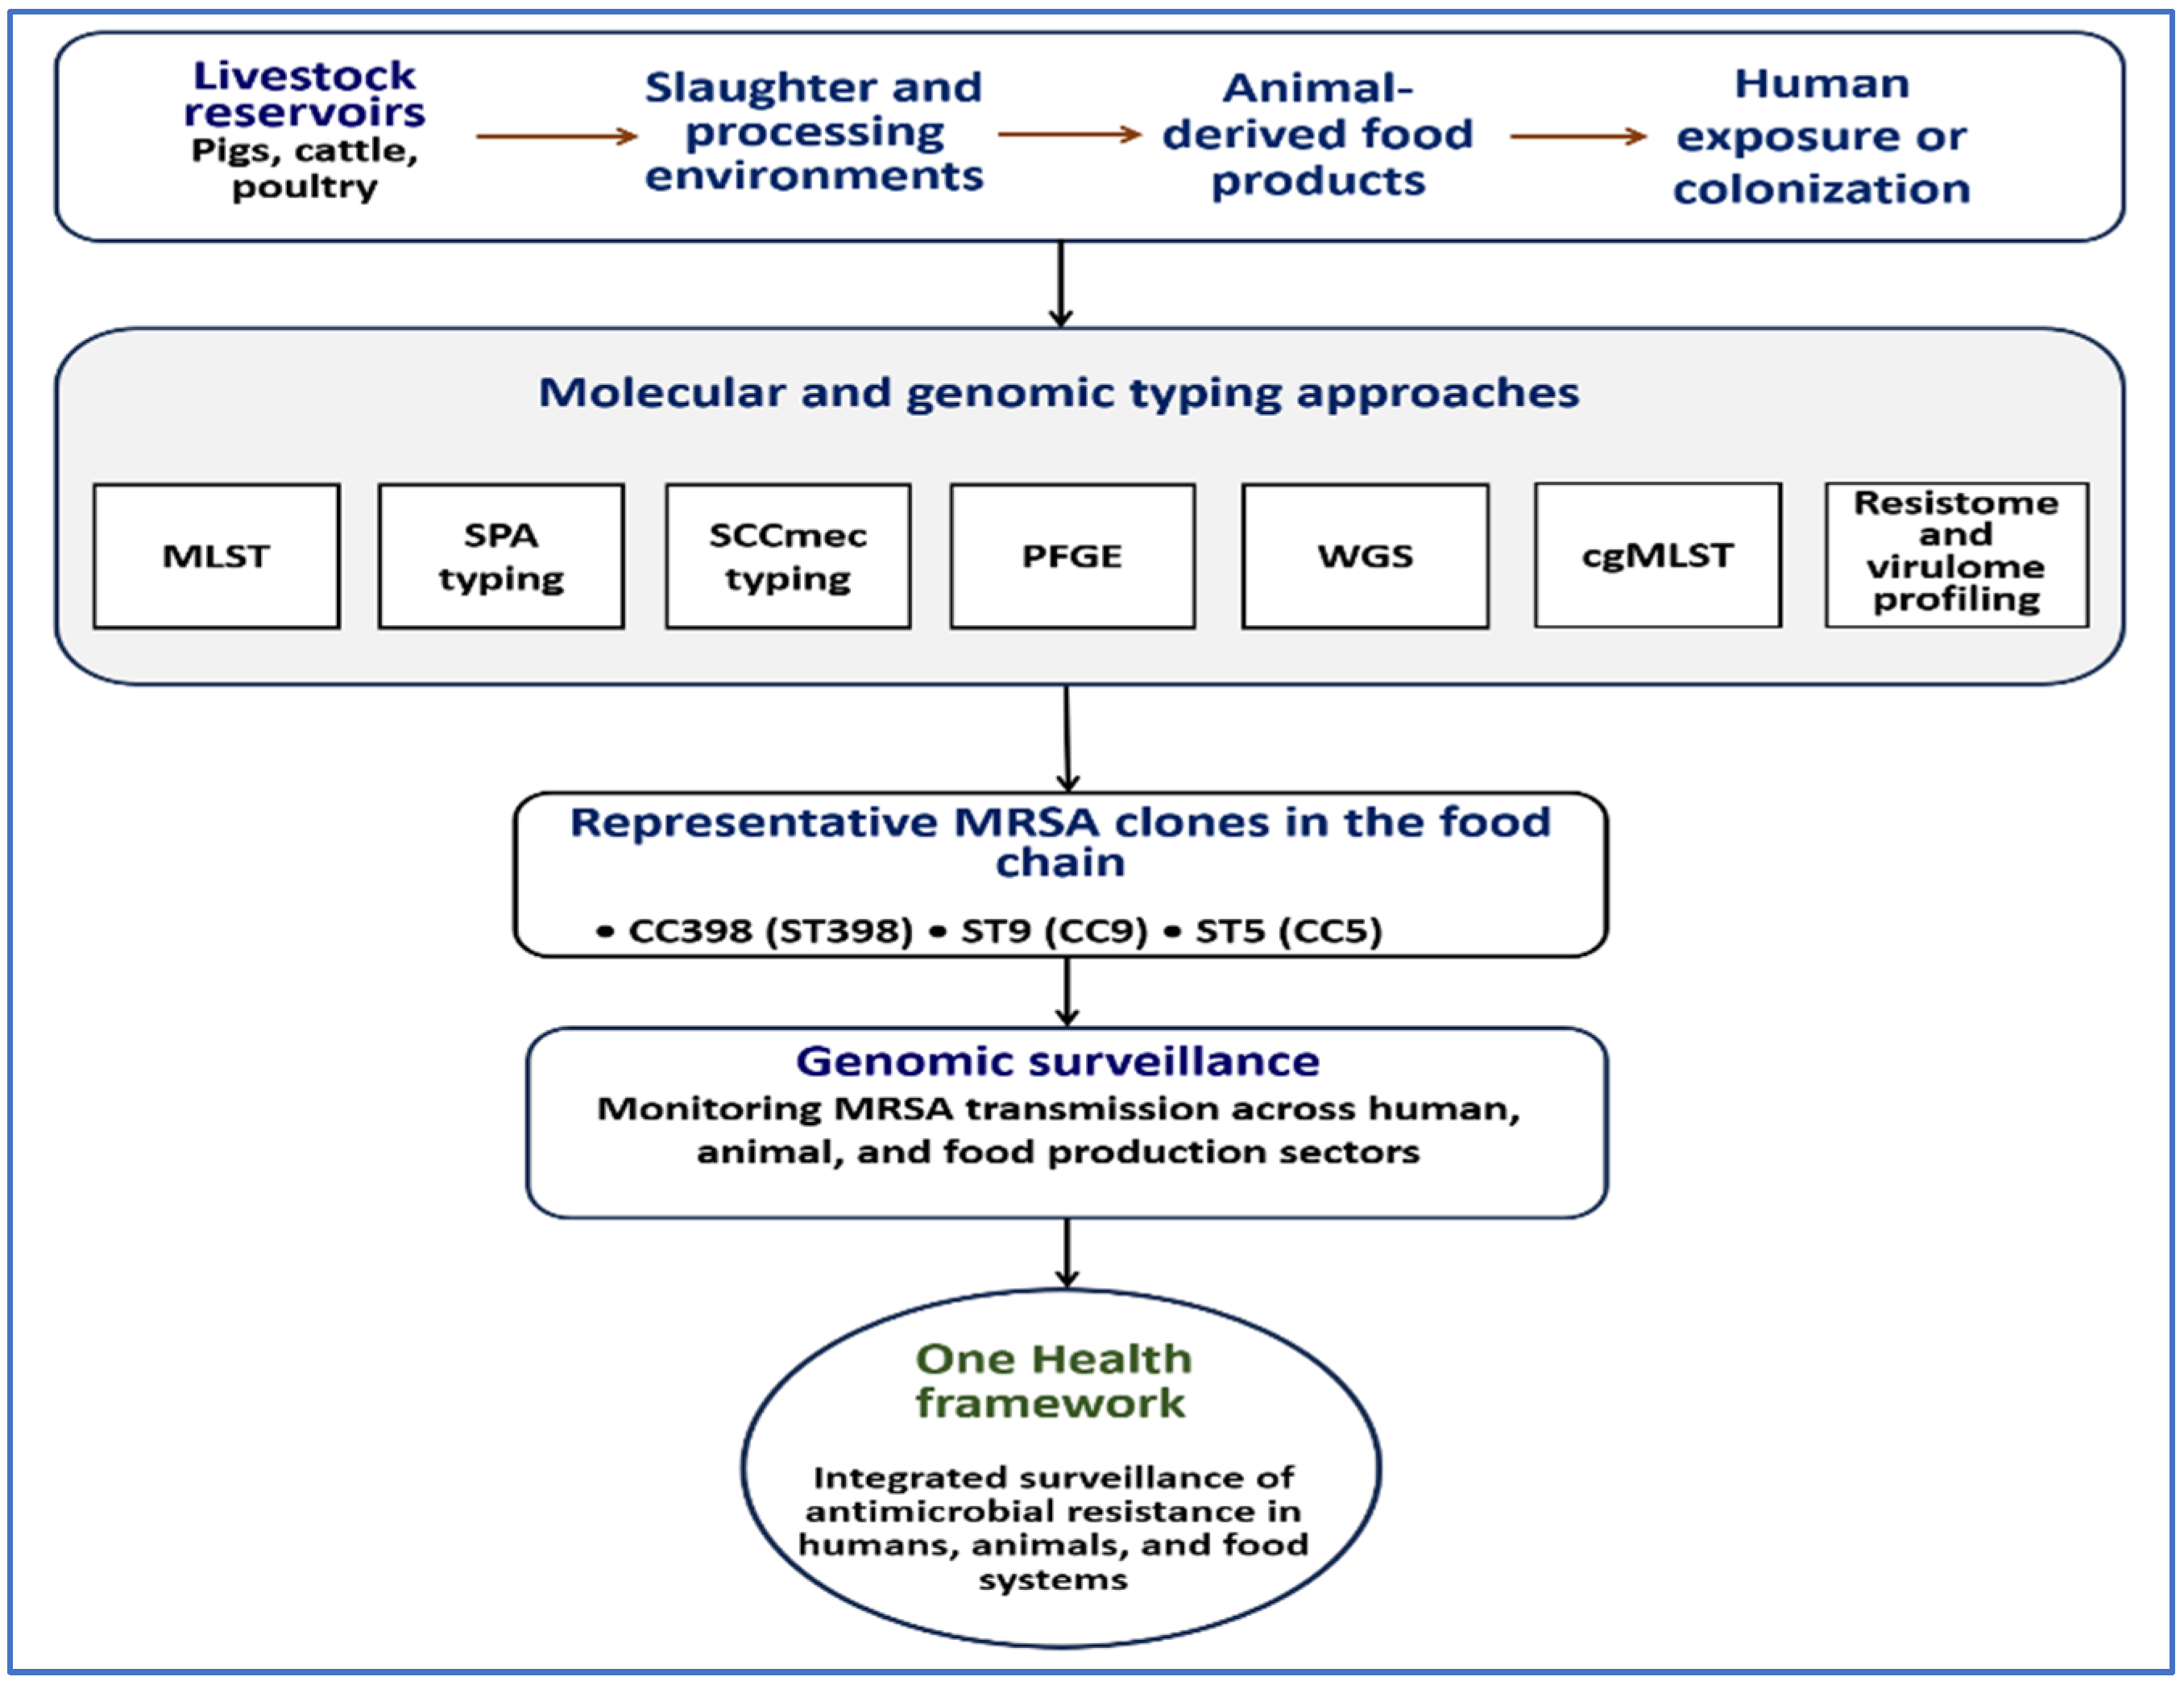
8. Molecular Epidemiology of Foodborne MRSA
8.1. Classical Molecular Typing Methods
8.2. Whole-Genome Sequencing (WGS) in MRSA Surveillance
8.3. Dominant MRSA Clones in the Food Chain

| Clone/Lineage | Primary Host | Geographic Distribution | Typical Spa Types | Common SCCmec Types | Key References |
|---|---|---|---|---|---|
| CC398 (ST398) | Pigs, cattle, poultry | Europe, North America, Asia | t011, t034 | IV, V | [26,90,145] |
| ST9 (CC9) | Pigs | East and Southeast Asia | t899 lineage variants | IV, V | [148,149] |
| ST5 (CC5) | Humans, livestock | Global | t002 and related types | II, IV | [47,150] |
| ST8 (CC8) | Humans; occasionally food products | North America | t008 | IV | [47,100] |
9. Virulence Determinants of Foodborne MRSA
9.1. Staphylococcal Enterotoxins
9.2. Panton–Valentine Leukocidin (PVL)
9.3. Biofilm Formation and Persistence
9.4. Surface Adhesins and Host Colonization
10. Transmission Pathways from the Food Chain to Humans
10.1. Occupational Exposure
10.2. Foodborne Exposure
10.3. Environmental Dissemination
11. Public Health Implications
12. Surveillance and Control Strategies
12.1. Integrated One Health Surveillance Systems
12.2. Antimicrobial Stewardship in Livestock Production
12.3. Hygiene and Food Safety Interventions
13. Future Perspectives and Research Priorities
14. Conclusions
Author Contributions
Funding
Institutional Review Board Statement
Informed Consent Statement
Data Availability Statement
Acknowledgments
Conflicts of Interest
References
- Prestinaci, F.; Pezzotti, P.; Pantosti, A. Antimicrobial resistance: A global multifaceted phenomenon. Pathog. Glob. Health 2015, 109, 309–318. [Google Scholar] [CrossRef] [Scilit]
- World Health Organization (WHO). Antimicrobial Resistance: Global Report on Surveillance; World Health Organization: Geneva, Switzerland, 2014; Available online: https://www.who.int/publications/i/item/9789241564748 (accessed on 15 February 2026).
- Ventola, C.L. The antibiotic resistance crisis: Part 1: Causes and threats. Pharm. Ther. 2015, 40, 277. [Google Scholar]
- Ferri, M.; Ranucci, E.; Romagnoli, P.; Giaccone, V. Antimicrobial resistance: A global emerging threat to public health systems. Crit. Rev. Food Sci. Nutr. 2017, 57, 2857–2876. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Salam, M.A.; Al-Amin, M.Y.; Salam, M.T.; Pawar, J.S.; Akhter, N.; Rabaan, A.A.; Alqumber, M.A. Antimicrobial resistance: A growing serious threat for global public health. Healthcare 2023, 11, 1946. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Okeke, I.N.; de Kraker, M.E.; Van Boeckel, T.P.; Kumar, C.K.; Schmitt, H.; Gales, A.C.; Bertagnolio, S.; Sharland, M.; Laxminarayan, R. The scope of the antimicrobial resistance challenge. Lancet 2024, 403, 2426–2438, Erratum in Lancet 2024, 404, 1018. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Murray, C.J.; Ikuta, K.S.; Sharara, F.; Swetschinski, L.; Aguilar, G.R.; Gray, A.; Han, C.; Bisignano, C.; Rao, P.; Wool, E. Global burden of bacterial antimicrobial resistance in 2019: A systematic analysis. Lancet 2022, 399, 629–655, Erratum in Lancet 2022, 400, 1102. [Google Scholar] [CrossRef] [Scilit]
- Tabassum, F.; Munir, A.; Shakeel, F.; Zia, T.; Khan, M.U.Z.; Tahir, Z. Methicillin resistance in Staphylococcus aureus: A review of the mecA gene and its role in antibiotic resistance. Indus J. Biosci. Res. 2025, 3, 2302. [Google Scholar] [CrossRef] [Scilit]
- Peacock, S.J.; Paterson, G.K. Mechanisms of methicillin resistance in Staphylococcus aureus. Annu. Rev. Biochem. 2015, 84, 577–601. [Google Scholar] [CrossRef] [Scilit]
- Abebe, A.A.; Birhanu, A.G. Methicillin resistant Staphylococcus aureus: Molecular mechanisms underlying drug resistance development and novel strategies to combat. Infect. Drug Resist. 2023, 16, 7641–7662. [Google Scholar]
- Lade, H.; Kim, J.-S. Molecular determinants of β-lactam resistance in methicillin-resistant Staphylococcus aureus (MRSA): An updated review. Antibiotics 2023, 12, 1362. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Lu, H.; Hu, G.; Liu, J.; Lian, S.; Pang, S.; Zhu, G.; Ding, X. Unmasking MRSA’s Armor: Molecular Mechanisms of Resistance and Pioneering Therapeutic Countermeasures. Microorganisms 2025, 13, 1928. [Google Scholar] [CrossRef] [Scilit]
- Turner, N.A.; Sharma-Kuinkel, B.K.; Maskarinec, S.A.; Eichenberger, E.M.; Shah, P.P.; Carugati, M.; Holland, T.L.; Fowler, V.G., Jr. Methicillin-resistant Staphylococcus aureus: An overview of basic and clinical research. Nat. Rev. Microbiol. 2019, 17, 203–218. [Google Scholar] [CrossRef] [Scilit]
- Silva, V.; Araújo, S.; Monteiro, A.; Eira, J.; Pereira, J.E.; Maltez, L.; Igrejas, G.; Lemsaddek, T.S.; Poeta, P. Staphylococcus aureus and MRSA in livestock: Antimicrobial resistance and genetic lineages. Microorganisms 2023, 11, 124. [Google Scholar] [CrossRef] [Scilit]
- Khairullah, A.R.; Kurniawan, S.C.; Effendi, M.H.; Sudjarwo, S.A.; Ramandinianto, S.C.; Widodo, A.; Riwu, K.H.P.; Silaen, O.S.M.; Rehman, S. A review of new emerging livestock-associated methicillin-resistant Staphylococcus aureus from pig farms. Vet. World 2023, 16, 46. [Google Scholar] [CrossRef] [Scilit]
- Xing, L.; Cheng, M.; Wang, S.; Jiang, J.; Li, T.; Zhang, X.; Yang, J.; Tian, Y.; Liu, W. Methicillin-resistant Staphylococcus aureus contamination in meat and meat products: A systematic review and meta-analysis. Front. Microbiol. 2025, 16, 1636622. [Google Scholar] [CrossRef] [Scilit]
- Habib, I.; Ghazawi, A.; Mohamed, M.-Y.I.; Lakshmi, G.B.; Nassar, R.; Monecke, S.; Ehricht, R.; Moradigaravand, D.; Everett, D.; Goering, R. Exploring human-to-food contamination potential: Genome-based analysis of diversity, toxin repertoire, and antimicrobial resistance of methicillin-resistant Staphylococcus aureus in United Arab Emirates retail meat. One Health 2025, 21, 101216. [Google Scholar] [CrossRef] [Scilit]
- Köck, R.; Schaumburg, F.; Mellmann, A.; Köksal, M.; Jurke, A.; Becker, K.; Friedrich, A.W. Livestock-associated methicillin-resistant Staphylococcus aureus (MRSA) as causes of human infection and colonization in Germany. PLoS ONE 2013, 8, e55040. [Google Scholar] [CrossRef] [Scilit]
- Kluytmans, J. Methicillin-resistant Staphylococcus aureus in food products: Cause for concern or case for complacency? Clin. Microbiol. Infect. 2010, 16, 11–15. [Google Scholar] [CrossRef] [Scilit]
- Jevons, M.P. “Celbenin”-resistant staphylococci. Br. Med. J. 1961, 1, 124–125. [Google Scholar] [CrossRef] [Scilit]
- Chambers, H.F.; DeLeo, F.R. Waves of resistance: Staphylococcus aureus in the antibiotic era. Nat. Rev. Microbiol. 2009, 7, 629–641. [Google Scholar] [CrossRef] [Scilit]
- Hiramatsu, K.; Katayama, Y.; Yuzawa, H.; Ito, T. Molecular genetics of methicillin-resistant Staphylococcus aureus. Int. J. Med. Microbiol. 2002, 292, 67–74. [Google Scholar] [CrossRef] [Scilit]
- International Working Group on the Classification of Staphylococcal Cassette Chromosome Elements (IWG-SCC). Classification of staphylococcal cassette chromosome mec (SCCmec): Guidelines for reporting novel SCCmec elements. Antimicrob. Agents Chemother. 2009, 53, 4961–4967. [CrossRef] [Scilit]
- Harris, S.R.; Feil, E.J.; Holden, M.T.; Quail, M.A.; Nickerson, E.K.; Chantratita, N.; Gardete, S.; Tavares, A.; Day, N.; Lindsay, J.A. Evolution of MRSA during hospital transmission and intercontinental spread. Science 2010, 327, 469–474. [Google Scholar] [CrossRef] [Scilit]
- Otto, M. Community-associated MRSA: What makes them special? Int. J. Med. Microbiol. 2013, 303, 324–330. [Google Scholar] [CrossRef] [Scilit]
- Smith, T.C.; Wardyn, S.E. Human infections with Staphylococcus aureus CC398. Curr. Environ. Health Rep. 2015, 2, 41–51. [Google Scholar] [CrossRef] [Scilit]
- Price, L.B.; Stegger, M.; Hasman, H.; Aziz, M.; Larsen, J.; Andersen, P.S.; Pearson, T.; Waters, A.E.; Foster, J.T.; Schupp, J.M. Staphylococcus aureus CC398: Host adaptation and emergence of methicillin resistance in livestock. mBio 2012, 3, e00305-11. [Google Scholar] [CrossRef] [Scilit]
- Graveland, H.; Duim, B.; Van Duijkeren, E.; Heederik, D.; Wagenaar, J.A. Livestock-associated methicillin-resistant Staphylococcus aureus in animals and humans. Int. J. Med. Microbiol. 2011, 301, 630–634. [Google Scholar] [CrossRef] [Scilit]
- Anjum, M.F.; Marco-Jimenez, F.; Duncan, D.; Marín, C.; Smith, R.P.; Evans, S.J. Livestock-associated methicillin-resistant Staphylococcus aureus from animals and animal products in the UK. Front. Microbiol. 2019, 10, 2136. [Google Scholar] [CrossRef] [Scilit]
- Butaye, P.; Argudín, M.; Smith, T. Livestock-associated MRSA and its current evolution. Curr. Clin. Microbiol. Rep. 2016, 3, 19–31. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Xie, L.; Huang, H.; Li, Z.; Li, G.; Liu, P.; Xiao, D.; Zhang, X.; Xiong, W.; Zeng, Z. Prevalence of livestock-associated MRSA ST398 in a swine slaughterhouse in Guangzhou, China. Front. Microbiol. 2022, 13, 914764. [Google Scholar] [CrossRef] [Scilit]
- Vestergaard, M.; Frees, D.; Ingmer, H. Antibiotic resistance and the MRSA problem. Microbiol. Spectr. 2019, 7. [Google Scholar] [CrossRef] [Scilit]
- Wielders, C.; Fluit, A.; Brisse, S.; Verhoef, J.; Schmitz, F. mecA gene is widely disseminated in Staphylococcus aureus population. J. Clin. Microbiol. 2002, 40, 3970–3975. [Google Scholar] [CrossRef] [Scilit]
- Shalaby, M.-A.W.; Dokla, E.M.; Serya, R.A.; Abouzid, K.A. Penicillin binding protein 2a: An overview and a medicinal chemistry perspective. Eur. J. Med. Chem. 2020, 199, 112312. [Google Scholar] [CrossRef] [Scilit]
- Fergestad, M.E.; Stamsås, G.A.; Morales Angeles, D.; Salehian, Z.; Wasteson, Y.; Kjos, M. Penicillin-binding protein PBP2a provides variable levels of protection toward different β-lactams in Staphylococcus aureus RN4220. Microbiologyopen 2020, 9, e1057. [Google Scholar]
- Niemeyer, D.M.; Pucci, M.J.; Thanassi, J.A.; Sharma, V.K.; Archer, G.L. Role of mecA transcriptional regulation in the phenotypic expression of methicillin resistance in Staphylococcus aureus. J. Bacteriol. 1996, 178, 5464–5471. [Google Scholar] [CrossRef] [Scilit]
- McKinney, T.K.; Sharma, V.K.; Craig, W.A.; Archer, G.L. Transcription of the gene mediating methicillin resistance in Staphylococcus aureus (mecA) is corepressed but not coinduced by cognate mecA and β-lactamase regulators. J. Bacteriol. 2001, 183, 6862–6868. [Google Scholar] [CrossRef] [Scilit]
- Oliveira, D.C.; De Lencastre, H. Methicillin-resistance in Staphylococcus aureus is not affected by the overexpression in trans of the mecA gene repressor: A surprising observation. PLoS ONE 2011, 6, e23287. [Google Scholar] [CrossRef] [Scilit]
- Harrison, E.M.; Paterson, G.K.; Holden, M.T.; Larsen, J.; Stegger, M.; Larsen, A.R.; Petersen, A.; Skov, R.L.; Christensen, J.M.; Bak Zeuthen, A. Whole genome sequencing identifies zoonotic transmission of MRSA isolates with the novel mecA homologue mecC. EMBO Mol. Med. 2013, 5, 509–515. [Google Scholar] [CrossRef] [Scilit]
- Paterson, G.K.; Harrison, E.M.; Holmes, M.A. The emergence of mecC methicillin-resistant Staphylococcus aureus. Trends Microbiol. 2014, 22, 42–47. [Google Scholar] [CrossRef] [Scilit]
- Kim, C.; Mwangi, M.; Chung, M.; Milheirço, C.; de Lencastre, H.; Tomasz, A. The mechanism of heterogeneous beta-lactam resistance in MRSA: Key role of the stringent stress response. PLoS ONE 2013, 8, e82814, Correction in PLoS ONE 2014, 9. [Google Scholar]
- Ambade, S.S.; Gupta, V.K.; Bhole, R.P.; Khedekar, P.B.; Chikhale, R.V. A review on five and six-membered heterocyclic compounds targeting the penicillin-binding protein 2 (PBP2A) of methicillin-resistant Staphylococcus aureus (MRSA). Molecules 2023, 28, 7008. [Google Scholar] [CrossRef] [Scilit]
- Rosado, P.C.; Marques, M.M.; Justino, G.C. Targeting MRSA penicillin-binding protein 2a: Structural insights, allosteric mechanisms, and the potential of adjuvant inhibitors. Biochem. Pharmacol. 2025, 239, 117048. [Google Scholar] [CrossRef] [Scilit]
- Loor-Giler, A.; Sanchez-Castro, C.; Puga-Torres, B.; Santander-Parra, S.; Nuñez, L. mecA and mecC Positive Strains of Staphylococcus aureus Detected and Isolated from Raw Milk of Ecuador. Antibiotics 2025, 14, 1255. [Google Scholar] [CrossRef] [Scilit]
- Maree, M.; Thi Nguyen, L.T.; Ohniwa, R.L.; Higashide, M.; Msadek, T.; Morikawa, K. Natural transformation allows transfer of SCCmec-mediated methicillin resistance in Staphylococcus aureus biofilms. Nat. Commun. 2022, 13, 2477. [Google Scholar] [CrossRef] [Scilit]
- Liu, J.; Chen, D.; Peters, B.M.; Li, L.; Li, B.; Xu, Z.; Shirliff, M.E. Staphylococcal chromosomal cassettes mec (SCCmec): A mobile genetic element in methicillin-resistant Staphylococcus aureus. Microb. Pathog. 2016, 101, 56–67. [Google Scholar] [CrossRef] [Scilit]
- Lakhundi, S.; Zhang, K. Methicillin-resistant Staphylococcus aureus: Molecular characterization, evolution, and epidemiology. Clin. Microbiol. Rev. 2018, 31, e00020-18. [Google Scholar] [CrossRef] [Scilit]
- Rohrer, S.; Berger-Bachi, B. FemABX peptidyl transferases: A link between branched-chain cell wall peptide formation and β-lactam resistance in gram-positive cocci. Antimicrob. Agents Chemother. 2003, 47, 837–846. [Google Scholar]
- Berger-Bächi, B.; Rohrer, S. Factors influencing methicillin resistance in staphylococci. Arch. Microbiol. 2002, 178, 165–171. [Google Scholar] [CrossRef] [Scilit]
- Cheung, A.L.; Nishina, K.A.; Trotonda, M.P.; Tamber, S. The SarA protein family of Staphylococcus aureus. Int. J. Biochem. Cell Biol. 2008, 40, 355–361. [Google Scholar]
- Malachowa, N.; DeLeo, F.R. Mobile genetic elements of Staphylococcus aureus. Cell. Mol. Life Sci. 2010, 67, 3057–3071. [Google Scholar] [CrossRef] [Scilit]
- Planet, P.J. Life after USA300: The rise and fall of a superbug. J. Infect. Dis. 2017, 215, S71–S77. [Google Scholar] [CrossRef] [Scilit]
- Deurenberg, R.H.; Stobberingh, E.E. The evolution of Staphylococcus aureus. Infect. Genet. Evol. 2008, 8, 747–763. [Google Scholar] [CrossRef] [Scilit]
- Mlynarczyk-Bonikowska, B.; Kowalewski, C.; Krolak-Ulinska, A.; Marusza, W. Molecular mechanisms of drug resistance in Staphylococcus aureus. Int. J. Mol. Sci. 2022, 23, 8088. [Google Scholar] [CrossRef] [Scilit]
- Brdová, D.; Ruml, T.; Viktorová, J. Mechanism of staphylococcal resistance to clinically relevant antibiotics. Drug Resist. Updates 2024, 77, 101147. [Google Scholar] [CrossRef] [Scilit]
- Zaghen, F.; Sora, V.M.; Meroni, G.; Laterza, G.; Martino, P.A.; Soggiu, A.; Bonizzi, L.; Zecconi, A. Epidemiology of antimicrobial resistance genes in Staphyloccocus aureus isolates from a public database in a one health perspective—Sample characteristics and isolates’ sources. Antibiotics 2023, 12, 1225. [Google Scholar] [CrossRef] [Scilit]
- Miklasińska-Majdanik, M. Mechanisms of resistance to macrolide antibiotics among Staphylococcus aureus. Antibiotics 2021, 10, 1406. [Google Scholar] [CrossRef] [Scilit]
- Mohammad, S.Q.; Awayid, H.S.; Zarrouk-Mahjoub, S.; Jallil, I.S. Molecular identification of erm A and erm B, erm C genes in methicillin-resistant Staphylococcus aureus isolates from burns patients and their association with multidrug resistance. Cell. Mol. Biol. 2025, 71, 112–117. [Google Scholar] [CrossRef] [Scilit]
- El-Banna, T.E.-S.; Sonbol, F.I.; Kamer, A.M.A.; Badr, S.A.M.M. Genetic diversity of macrolides resistant Staphylococcus aureus clinical isolates and the potential synergistic effect of vitamins, C and K3. BMC Microbiol. 2024, 24, 30. [Google Scholar] [CrossRef] [Scilit]
- Yao, W.; Xu, G.; Li, D.; Bai, B.; Wang, H.; Cheng, H.; Zheng, J.; Sun, X.; Lin, Z.; Deng, Q. Staphylococcus aureus with an erm-mediated constitutive macrolide-lincosamide-streptogramin B resistance phenotype has reduced susceptibility to the new ketolide, solithromycin. BMC Infect. Dis. 2019, 19, 175. [Google Scholar] [CrossRef] [Scilit]
- Gherardi, G.; De Florio, L.; Lorino, G.; Fico, L.; Dicuonzo, G. Macrolide resistance genotypes and phenotypes among erythromycin-resistant clinical isolates of Staphylococcus aureus and coagulase-negative staphylococci, Italy. FEMS Immunol. Med. Microbiol. 2009, 55, 62–67. [Google Scholar] [CrossRef] [Scilit]
- Pinheiro, P.G.; Santiago, G.M.P.; da Silva, F.E.F.; de Araújo, A.C.J.; de Oliveira, C.R.T.; Freitas, P.R.; Rocha, J.E.; de Araújo Neto, J.B.; da Silva, M.M.C.; Tintino, S.R. Ferulic acid derivatives inhibiting Staphylococcus aureus tetK and MsrA efflux pumps. Biotechnol. Rep. 2022, 34, e00717. [Google Scholar]
- Dashtbani-Roozbehani, A.; Brown, M.H. Efflux pump mediated antimicrobial resistance by staphylococci in health-related environments: Challenges and the quest for inhibition. Antibiotics 2021, 10, 1502. [Google Scholar] [CrossRef] [Scilit]
- Lade, H.; Joo, H.-S.; Kim, J.-S. Molecular basis of non-β-lactam antibiotics resistance in Staphylococcus aureus. Antibiotics 2022, 11, 1378. [Google Scholar]
- Kaatz, G.W.; Seo, S.M.; Ruble, C.A. Mechanisms of fluoroquinolone resistance in Staphylococcus aureus. J. Infect. Dis. 1991, 163, 1080–1086. [Google Scholar] [CrossRef] [Scilit]
- Hooper, D.C. Emerging mechanisms of fluoroquinolone resistance. Emerg. Infect. Dis. 2001, 7, 337. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Piddock, L.J. Mechanisms of fluoroquinolone resistance: An update 1994–1998. Drugs 1999, 58, 11–18. [Google Scholar] [CrossRef] [Scilit]
- Atta, S.E.; Ghannawi, L.; Shakir, O.Y.; Gharab, K.M. Molecular investigation of gyrA mutations in clinical isolates of methicillin-resistant Staphylococcus aureus derived from diverse sources. Al-Rafidain J. Med. Sci. 2023, 5, S64–S70. [Google Scholar] [CrossRef] [Scilit]
- Poole, K. Efflux-mediated resistance to fluoroquinolones in gram-positive bacteria and the mycobacteria. Antimicrob. Agents Chemother. 2000, 44, 2595–2599. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tanaka, M.; Wang, T.; Onodera, Y.; Uchida, Y.; Sato, K. Mechanism of quinolone resistance in Staphylococcus aureus. J. Infect. Chemother. 2000, 6, 131–139. [Google Scholar] [CrossRef] [Scilit]
- Horii, T.; Suzuki, Y.; Monji, A.; Morita, M.; Muramatsu, H.; Kondo, Y.; Doi, M.; Takeshita, A.; Kanno, T.; Maekawa, M. Detection of mutations in quinolone resistance-determining regions in levofloxacin-and methicillin-resistant Staphylococcus aureus: Effects of the mutations on fluoroquinolone MICs. Diagn. Microbiol. Infect. Dis. 2003, 46, 139–145. [Google Scholar]
- Costa, S.S.; Junqueira, E.; Palma, C.; Viveiros, M.; Melo-Cristino, J.; Amaral, L.; Couto, I. Resistance to antimicrobials mediated by efflux pumps in Staphylococcus aureus. Antibiotics 2013, 2, 83–99. [Google Scholar] [CrossRef] [Scilit]
- Rajput, P.; Nahar, K.S.; Rahman, K.M. Evaluation of antibiotic resistance mechanisms in gram-positive bacteria. Antibiotics 2024, 13, 1197. [Google Scholar] [CrossRef] [Scilit]
- Sinha, S.; Aggarwal, S.; Singh, D.V. Efflux pumps: Gatekeepers of antibiotic resistance in Staphylococcus aureus biofilms. Microb. Cell 2024, 11, 368. [Google Scholar]
- Lekshmi, M.; Ammini, P.; Adjei, J.; Sanford, L.M.; Shrestha, U.; Kumar, S.; Varela, M.F. Modulation of antimicrobial efflux pumps of the major facilitator superfamily in Staphylococcus aureus. AIMS Microbiol. 2018, 4, 1–18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Costa, R.H.S.d.; Pessoa, R.T.; Silva, E.d.S.; Araujo, I.M.; Gonçalves, S.A.; Rocha, J.E.; Pereira Junior, F.N.; Oliveira, N.C.; Oliveira, V.M.d.; Rocha, M.N.d. Antibacterial and Inhibitory Activity of Nora and Mepa Efflux Pumps of Estragole Complexed to β-Cyclodextrin (ES/β-CD) In Vitro Against Staphylococcus aureus Bacteria, Molecular Docking and MPO-Based Pharmacokinetics Prediction. Pharmaceutics 2024, 16, 1469. [Google Scholar] [CrossRef] [Scilit]
- Zimmermann, S.; Klinger-Strobel, M.; Bohnert, J.A.; Wendler, S.; Rödel, J.; Pletz, M.W.; Löffler, B.; Tuchscherr, L. Clinically approved drugs inhibit the Staphylococcus aureus multidrug NorA efflux pump and reduce biofilm formation. Front. Microbiol. 2019, 10, 2762. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ika Irianti, M.; Vincken, J.-P.; Van Dinteren, S.; Ter Beest, E.; Pos, K.M.; Araya-Cloutier, C. Prenylated isoflavonoids from Fabaceae against the NorA efflux pump in Staphylococcus aureus. Sci. Rep. 2023, 13, 22548. [Google Scholar] [CrossRef] [Scilit]
- Hassanzadeh, S.; Pourmand, M.R.; Mashhadi, R.; Ghazvini, K. Epidemiology of efflux pumps genes mediating resistance among Staphylococcus aureus; A systematic review. Microb. Pathog. 2020, 139, 103850. [Google Scholar] [CrossRef] [Scilit]
- Sharma, A.; Gupta, V.K.; Pathania, R. Efflux pump inhibitors for bacterial pathogens: From bench to bedside. Indian J. Med. Res. 2019, 149, 129–145. [Google Scholar] [CrossRef] [Scilit]
- Mitchell, B.A.; Brown, M.H.; Skurray, R.A. QacA multidrug efflux pump from Staphylococcus aureus: Comparative analysis of resistance to diamidines, biguanidines, and guanylhydrazones. Antimicrob. Agents Chemother. 1998, 42, 475–477. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Buffet-Bataillon, S.; Tattevin, P.; Bonnaure-Mallet, M.; Jolivet-Gougeon, A. Emergence of resistance to antibacterial agents: The role of quaternary ammonium compounds—A critical review. Int. J. Antimicrob. Agents 2012, 39, 381–389. [Google Scholar] [CrossRef] [Scilit]
- Foster, T.J. Antibiotic resistance in Staphylococcus aureus. Current status and future prospects. FEMS Microbiol. Rev. 2017, 41, 430–449. [Google Scholar] [CrossRef] [Scilit]
- Roberts, M.C. Update on macrolide–lincosamide–streptogramin, ketolide, and oxazolidinone resistance genes. FEMS Microbiol. Lett. 2008, 282, 147–159. [Google Scholar]
- Wendlandt, S.; Li, B.; Ma, Z.; Schwarz, S. Complete sequence of the multi-resistance plasmid pV7037 from a porcine methicillin-resistant Staphylococcus aureus. Vet. Microbiol. 2013, 166, 650–654. [Google Scholar]
- Chopra, I.; Roberts, M. Tetracycline antibiotics: Mode of action, applications, molecular biology, and epidemiology of bacterial resistance. Microbiol. Mol. Biol. Rev. 2001, 65, 232–260. [Google Scholar] [CrossRef] [Scilit]
- Hooper, D.C.; Jacoby, G.A. Topoisomerase inhibitors: Fluoroquinolone mechanisms of action and resistance. Cold Spring Harb. Perspect. Med. 2016, 6, a025320. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kaatz, G.W.; McAleese, F.; Seo, S.M. Multidrug resistance in Staphylococcus aureus due to overexpression of a novel multidrug and toxin extrusion (MATE) transport protein. Antimicrob. Agents Chemother. 2005, 49, 1857–1864. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Golob, M.; Pate, M.; Kušar, D.; Zajc, U.; Papić, B.; Ocepek, M.; Zdovc, I.; Avberšek, J. Antimicrobial resistance and molecular characterization of methicillin-resistant Staphylococcus aureus from two pig farms: Longitudinal study of LA-MRSA. Antibiotics 2022, 11, 1532. [Google Scholar] [CrossRef] [Scilit]
- Silva, V.; Monteiro, A.; Pereira, J.E.; Maltez, L.; Igrejas, G.; Poeta, P. MRSA in humans, pets and livestock in Portugal: Where we came from and where we are going. Pathogens 2022, 11, 1110. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, C.; Wu, F. Livestock-associated methicillin-resistant Staphylococcus aureus (LA-MRSA) colonisation and infection among livestock workers and veterinarians: A systematic review and meta-analysis. Occup. Environ. Med. 2021, 78, 530–540. [Google Scholar] [CrossRef] [Scilit]
- Madsen, A.M.; Kurdi, I.; Feld, L.; Tendal, K. Airborne MRSA and total Staphylococcus aureus as associated with particles of different sizes on pig farms. Ann. Work Expo. Health 2018, 62, 966–977. [Google Scholar]
- Pedersen, K.; Nielsen, M.W.; Fertner, M.E.; Espinosa-Gongora, C.; Bækbo, P. Development of Livestock-Associated Methicillin-Resistant Staphylococcus aureus (LA-MRSA) Loads in Pigs and Pig Stables During the Fattening Period. Vet. Sci. 2024, 11, 558. [Google Scholar] [CrossRef] [Scilit]
- Sadiq, A.; Samad, M.; Saddam; Basharat, N.; Ali, S.; Roohullah; Saad, Z.; Khan, A.N.; Ahmad, Y.; Khan, A. Methicillin-resistant Staphylococcus aureus (MRSA) in slaughter houses and meat shops in capital territory of Pakistan during 2018–2019. Front. Microbiol. 2020, 11, 577707. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Di Ciccio, P.; Vergara, A.; Festino, A.R.; Paludi, D.; Zanardi, E.; Ghidini, S.; Ianieri, A. Biofilm formation by Staphylococcus aureus on food contact surfaces: Relationship with temperature and cell surface hydrophobicity. Food Control 2015, 50, 930–936. [Google Scholar] [CrossRef] [Scilit]
- Shen, J.; Wang, H.; Zhu, C.; Zhang, M.; Shang, F.; Xue, T. Effect of biofilm on the survival of Staphylococcus aureus isolated from raw milk in high temperature and drying environment. Food Res. Int. 2021, 149, 110672. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pérez-Boto, D.; D’Arrigo, M.; García-Lafuente, A.; Bravo, D.; Pérez-Baltar, A.; Gaya, P.; Medina, M.; Arqués, J.L. Staphylococcus aureus in the processing environment of cured meat products. Foods 2023, 12, 2161. [Google Scholar] [CrossRef] [Scilit]
- Song, M.; Tang, Q.; Ding, Y.; Tan, P.; Zhang, Y.; Wang, T.; Zhou, C.; Xu, S.; Lyu, M.; Bai, Y. Staphylococcus aureus and biofilms: Transmission, threats, and promising strategies in animal husbandry. J. Anim. Sci. Biotechnol. 2024, 15, 44. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- de Boer, E.; Zwartkruis-Nahuis, J.; Wit, B.; Huijsdens, X.; De Neeling, A.; Bosch, T.; Van Oosterom, R.; Vila, A.; Heuvelink, A. Prevalence of methicillin-resistant Staphylococcus aureus in meat. Int. J. Food Microbiol. 2009, 134, 52–56. [Google Scholar] [CrossRef] [Scilit]
- Waters, A.E.; Contente-Cuomo, T.; Buchhagen, J.; Liu, C.M.; Watson, L.; Pearce, K.; Foster, J.T.; Bowers, J.; Driebe, E.M.; Engelthaler, D.M. Multidrug-resistant Staphylococcus aureus in US meat and poultry. Clin. Infect. Dis. 2011, 52, 1227–1230. [Google Scholar] [CrossRef] [Scilit]
- Wu, S.; Huang, J.; Wu, Q.; Zhang, J.; Zhang, F.; Yang, X.; Wu, H.; Zeng, H.; Chen, M.; Ding, Y. Staphylococcus aureus isolated from retail meat and meat products in China: Incidence, antibiotic resistance and genetic diversity. Front. Microbiol. 2018, 9, 2767. [Google Scholar] [CrossRef] [Scilit]
- Fetsch, A.; Contzen, M.; Hartelt, K.; Kleiser, A.; Maassen, S.; Rau, J.; Kraushaar, B.; Layer, F.; Strommenger, B. Staphylococcus aureus food-poisoning outbreak associated with the consumption of ice-cream. Int. J. Food Microbiol. 2014, 187, 1–6. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Normanno, G.; Corrente, M.; La Salandra, G.; Dambrosio, A.; Quaglia, N.C.; Parisi, A.; Greco, G.; Bellacicco, A.; Virgilio, S.; Celano, G.V. Methicillin-resistant Staphylococcus aureus (MRSA) in foods of animal origin product in Italy. Int. J. Food Microbiol. 2007, 117, 219–222. [Google Scholar] [CrossRef] [Scilit]
- Hanson, B.; Dressler, A.; Harper, A.; Scheibel, R.; Wardyn, S.; Roberts, L.; Kroeger, J.; Smith, T. Prevalence of Staphylococcus aureus and methicillin-resistant Staphylococcus aureus (MRSA) on retail meat in Iowa. J. Infect. Public Health 2011, 4, 169–174. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.; Li, G.; Xia, X.; Yang, B.; Xi, M.; Meng, J. Antimicrobial susceptibility and molecular typing of methicillin-resistant Staphylococcus aureus in retail foods in Shaanxi, China. Foodborne Pathog. Dis. 2014, 11, 281–286. [Google Scholar] [CrossRef] [Scilit]
- Jamali, H.; Paydar, M.; Radmehr, B.; Ismail, S.; Dadrasnia, A. Prevalence and antimicrobial resistance of Staphylococcus aureus isolated from raw milk and dairy products. Food Control 2015, 54, 383–388. [Google Scholar] [CrossRef] [Scilit]
- Oniciuc, E.A.; Likotrafiti, E.; Alvarez-Molina, A.; Prieto, M.; Santos, J.A.; Alvarez-Ordóñez, A. The present and future of whole genome sequencing (WGS) and whole metagenome sequencing (WMS) for surveillance of antimicrobial resistant microorganisms and antimicrobial resistance genes across the food chain. Genes 2018, 9, 268, Correction in Genes 2018, 9, 315. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Oniciuc, E.-A.; Likotrafiti, E.; Alvarez-Molina, A.; Prieto, M.; López, M.; Alvarez-Ordóñez, A. Food processing as a risk factor for antimicrobial resistance spread along the food chain. Curr. Opin. Food Sci. 2019, 30, 21–26. [Google Scholar] [CrossRef] [Scilit]
- Algammal, A.M.; Hetta, H.F.; Elkelish, A.; Alkhalifah, D.H.H.; Hozzein, W.N.; Batiha, G.E.-S.; El Nahhas, N.; Mabrok, M.A. Methicillin-Resistant Staphylococcus aureus (MRSA): One health perspective approach to the bacterium epidemiology, virulence factors, antibiotic-resistance, and zoonotic impact. Infect. Drug Resist. 2020, 13, 3255–3265. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Abdullahi, I.N.; Lozano, C.; Ruiz-Ripa, L.; Fernández-Fernández, R.; Zarazaga, M.; Torres, C. Ecology and genetic lineages of nasal Staphylococcus aureus and MRSA carriage in healthy persons with or without animal-related occupational risks of colonization: A review of global reports. Pathogens 2021, 10, 1000. [Google Scholar] [CrossRef] [Scilit]
- Bal, A.; Coombs, G.; Holden, M.; Lindsay, J.; Nimmo, G.; Tattevin, P.; Skov, R. Genomic insights into the emergence and spread of international clones of healthcare-, community-and livestock-associated meticillin-resistant Staphylococcus aureus: Blurring of the traditional definitions. J. Glob. Antimicrob. Resist. 2016, 6, 95–101. [Google Scholar] [CrossRef] [Scilit]
- Kumar, S.; Anwer, R.; Yadav, M.; Sehrawat, N.; Singh, M.; Kumar, V. Molecular typing and global epidemiology of Staphylococcus aureus. Curr. Pharmacol. Rep. 2021, 7, 179–186. [Google Scholar] [CrossRef] [Scilit]
- Mehndiratta, P.; Bhalla, P. Typing of Methicillin resistant Staphylococcus aureus: A technical review. Indian J. Med. Microbiol. 2012, 30, 16–23. [Google Scholar] [CrossRef] [Scilit]
- Maeda, R.; Kobayashi, H.; Higashidani, M.; Matsuhisa, T.; Sawa, A.; Miyake, K.; Tayama, Y.; Kimura, K.; Itoh, H.; Okano, T. Molecular epidemiological and pharmaceutical studies of methicillin-resistant Staphylococcus aureus isolated at hospitals in Kure City, Japan. Access Microbiol. 2022, 4, 000319. [Google Scholar] [CrossRef] [Scilit]
- Shokoohizadeh, L.; Dehghani, T.; NamordiZadeh, V.; Karmostaji, A. New sequence types of Staphylococcus aureus strains isolated from hospitals and community settings in southern Iran. Jundishapur J. Microbiol. 2024, 17, e144398. [Google Scholar] [CrossRef] [Scilit]
- Faria, N.A.; Carrico, J.A.; Oliveira, D.C.; Ramirez, M.; De Lencastre, H. Analysis of typing methods for epidemiological surveillance of both methicillin-resistant and methicillin-susceptible Staphylococcus aureus strains. J. Clin. Microbiol. 2008, 46, 136–144. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hallin, M.; Deplano, A.; Struelens, M.J. Molecular typing of bacterial pathogens: A tool for the epidemiological study and control of infectious diseases. In New Frontiers of Molecular Epidemiology of Infectious Diseases; Morand, S., Beaudeau, F., Cabaret, J., Eds.; Springer: Dordrecht, The Netherlands, 2011; pp. 9–25. [Google Scholar]
- Enright, M.C.; Day, N.P.; Davies, C.E.; Peacock, S.J.; Spratt, B.G. Multilocus sequence typing for characterization of methicillin-resistant and methicillin-susceptible clones of Staphylococcus aureus. J. Clin. Microbiol. 2000, 38, 1008–1015. [Google Scholar] [CrossRef] [Scilit]
- Maiden, M.C.; Bygraves, J.A.; Feil, E.; Morelli, G.; Russell, J.E.; Urwin, R.; Zhang, Q.; Zhou, J.; Zurth, K.; Caugant, D.A. Multilocus sequence typing: A portable approach to the identification of clones within populations of pathogenic microorganisms. Proc. Natl. Acad. Sci. USA 1998, 95, 3140–3145. [Google Scholar] [CrossRef] [Scilit]
- Feil, E.J.; Li, B.C.; Aanensen, D.M.; Hanage, W.P.; Spratt, B.G. eBURST: Inferring patterns of evolutionary descent among clusters of related bacterial genotypes from multilocus sequence typing data. J. Bacteriol. 2004, 186, 1518–1530. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Harmsen, D.; Claus, H.; Witte, W.; Rothganger, J.; Claus, H.; Turnwald, D.; Vogel, U. Typing of methicillin-resistant Staphylococcus aureus in a university hospital setting by using novel software for spa repeat determination and database management. J. Clin. Microbiol. 2003, 41, 5442–5448. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shopsin, B.; Gomez, M.; Montgomery, S.; Smith, D.; Waddington, M.; Dodge, D.; Bost, D.; Riehman, M.; Naidich, S.; Kreiswirth, B. Evaluation of protein A gene polymorphic region DNA sequencing for typing of Staphylococcus aureus strains. J. Clin. Microbiol. 1999, 37, 3556–3563. [Google Scholar] [CrossRef] [Scilit]
- Oumarou, Z.; Henri, O.S.; Nestor, I.H.; Francois, T.; Aly, S. History, Structure, Epidemiology and Molecular Typing of Staphylococcal Cassette Chromosomes Mec (Sccmec) involved in Multiple Resistances to Beta-Lactams in the Genus Staphylococcus: An Overview. Arch. Clin. Biomed. Res. 2022, 6, 791–799. [Google Scholar] [CrossRef] [Scilit]
- Abdulgader, S.M.; Shittu, A.O.; Nicol, M.P.; Kaba, M. Molecular epidemiology of Methicillin-resistant Staphylococcus aureus in Africa: A systematic review. Front. Microbiol. 2015, 6, 348. [Google Scholar] [CrossRef] [Scilit]
- Tenover, F.C.; Arbeit, R.D.; Goering, R.V.; Mickelsen, P.A.; Murray, B.E.; Persing, D.H.; Swaminathan, B. Interpreting chromosomal DNA restriction patterns produced by pulsed-field gel electrophoresis: Criteria for bacterial strain typing. J. Clin. Microbiol. 1995, 33, 2233–2239. [Google Scholar] [CrossRef] [Scilit]
- Murchan, S.; Kaufmann, M.E.; Deplano, A.; de Ryck, R.; Struelens, M.; Zinn, C.E.; Fussing, V.; Salmenlinna, S.; Vuopio-Varkila, J.; El Solh, N. Harmonization of pulsed-field gel electrophoresis protocols for epidemiological typing of strains of methicillin-resistant Staphylococcus aureus: A single approach developed by consensus in 10 European laboratories and its application for tracing the spread of related strains. J. Clin. Microbiol. 2003, 41, 1574–1585. [Google Scholar]
- Güven Gökmen, T.; Kalayci, Y.; Yaman, A.; Köksal, F. Molecular characterization of methicillin-resistant Staphylococcus aureus strains by spa typing and pulsed field gel electrophoresis methods. BMC Microbiol. 2018, 18, 155. [Google Scholar] [CrossRef] [Scilit]
- Coleman, D.C.; Shore, A.C.; Goering, R.V.; Monecke, S. New insights and updates on the molecular epidemiology and antimicrobial resistance of MRSA in humans in the whole-genome sequencing era. Front. Microbiol. 2019, 10, 637. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Humphreys, H.; Coleman, D. Contribution of whole-genome sequencing to understanding of the epidemiology and control of meticillin-resistant Staphylococcus aureus. J. Hosp. Infect. 2019, 102, 189–199. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, H.; Tian, L.; Chen, T.; Chen, W.; Ge, Y.; Bi, J.; Fang, Z.; Chen, M. Prevalence and WGS-based characteristics of MRSA isolates in hospitals in Shanghai, China. Front. Microbiol. 2022, 13, 1002691. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Salipante, S.J.; SenGupta, D.J.; Cummings, L.A.; Land, T.A.; Hoogestraat, D.R.; Cookson, B.T. Application of whole-genome sequencing for bacterial strain typing in molecular epidemiology. J. Clin. Microbiol. 2015, 53, 1072–1079. [Google Scholar] [CrossRef] [Scilit]
- Ullah, N.; Dar, H.A.; Naz, K.; Andleeb, S.; Rahman, A.; Saeed, M.T.; Hanan, F.; Bae, T.; Ali, A. Genomic investigation of methicillin-resistant Staphylococcus aureus ST113 strains isolated from tertiary care hospitals in Pakistan. Antibiotics 2021, 10, 1121. [Google Scholar] [CrossRef] [Scilit]
- Kim, D.-H.; Han, D.-G.; Lee, S.; Yoo, J.-S.; Jeon, S.-M. Comparative Genomic and Epidemiologic Analysis of Methicillin-Resistant Staphylococcus aureus Isolates in Republic of Korea. Antibiotics 2026, 15, 235. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cho, H.; Kim, Y.; Jang, B.; Park, K.T. Clonal distribution of livestock-associated methicillin-resistant Staphylococcus aureus in pig farms of Korea: Emergence of a novel variant staphylococcal chromosome cassette mec. Int. J. Food Microbiol. 2025, 441, 111341. [Google Scholar] [CrossRef] [Scilit]
- Aanensen, D.M.; Feil, E.J.; Holden, M.T.; Dordel, J.; Yeats, C.A.; Fedosejev, A.; Goater, R.; Castillo-Ramírez, S.; Corander, J.; Colijn, C. Whole-genome sequencing for routine pathogen surveillance in public health: A population snapshot of invasive Staphylococcus aureus in Europe. mBio 2016, 7, e00444-16. [Google Scholar] [CrossRef] [Scilit]
- Echaniz-Avilés, G.; Núñez-García, L.Á.; Rodríguez-Noriega, E.; Velázquez-Acosta, C.; López-Jácome, L.E.; López-Gutiérrez, E.; Pérez-Vicelis, T.; Torres-Báez, C.; Garza-Ramos, U.; Rodríguez-Medina, N. Genomic characteristics and molecular epidemiology of MRSA from medical centers in Mexico: Results from the Invifar network. PLoS ONE 2025, 20, e0317284. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tang, Y.; Larsen, J.; Kjeldgaard, J.; Andersen, P.S.; Skov, R.; Ingmer, H. Methicillin-resistant and-susceptible Staphylococcus aureus from retail meat in Denmark. Int. J. Food Microbiol. 2017, 249, 72–76. [Google Scholar] [CrossRef] [Scilit]
- Sieber, R.N.; Skov, R.L.; Nielsen, J.; Schulz, J.; Price, L.B.; Aarestrup, F.M.; Larsen, A.R.; Stegger, M.; Larsen, J. Drivers and dynamics of methicillin-resistant livestock-associated Staphylococcus aureus CC398 in pigs and humans in Denmark. mBio 2018, 9, e02142-18. [Google Scholar] [CrossRef] [Scilit]
- Kong, Z.; Zhao, P.; Liu, H.; Yu, X.; Qin, Y.; Su, Z.; Wang, S.; Xu, H.; Chen, J. Whole-genome sequencing for the investigation of a hospital outbreak of MRSA in China. PLoS ONE 2016, 11, e0149844. [Google Scholar] [CrossRef] [Scilit]
- Soliman, M.S.; Soliman, N.S.; El-Manakhly, A.R.; ElBanna, S.A.; Aziz, R.K.; El-Kholy, A.A. Genomic characterization of methicillin-resistant Staphylococcus aureus (MRSA) by high-throughput sequencing in a tertiary care hospital. Genes 2020, 11, 1219. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Silva, V.; Silva, A.; Barbero, R.; Romero, M.; Del Campo, R.; Caniça, M.; Cordeiro, R.; Igrejas, G.; Poeta, P. Resistome, Virulome, and Clonal Variation in Methicillin-Resistant Staphylococcus aureus (MRSA) in Healthy Swine Populations: A Cross-Sectional Study. Genes 2024, 15, 532. [Google Scholar] [CrossRef] [Scilit]
- González, M.J.; Parada, J.; Blasko, E.; Sosa, E.J.; Suleyman, G.; Kaur, J.; Maki, G.; Prentiss, T.; Corti Isgro, M.; Pereyra, N. Phylogenomic insights into LA-MRSA from Argentine pig farm environments: Novel OptrA variant and regional emergence of an ST9 lineage co-circulating with international CC398 lineages. Front. Microbiol. 2025, 16, 1662779. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Catry, B.; Van Duijkeren, E.; Pomba, M.; Greko, C.; Moreno, M.; Pyörälä, S.; Ružauskas, M.; Sanders, P.; Threlfall, E.; Ungemach, F. Reflection paper on MRSA in food-producing and companion animals: Epidemiology and control options for human and animal health. Epidemiol. Infect. 2010, 138, 626–644. [Google Scholar] [CrossRef] [Scilit]
- Sharma, M.; Nunez-Garcia, J.; Kearns, A.M.; Doumith, M.; Butaye, P.R.; Argudín, M.A.; Lahuerta-Marin, A.; Pichon, B.; AbuOun, M.; Rogers, J. Livestock-associated methicillin resistant Staphylococcus aureus (LA-MRSA) clonal complex (CC) 398 isolated from UK animals belong to European lineages. Front. Microbiol. 2016, 7, 1741. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Verkade, E.; Kluytmans, J. Livestock-associated Staphylococcus aureus CC398: Animal reservoirs and human infections. Infect. Genet. Evol. 2014, 21, 523–530. [Google Scholar] [CrossRef] [Scilit]
- Pantosti, A. Methicillin-resistant Staphylococcus aureus associated with animals and its relevance to human health. Front. Microbiol. 2012, 3, 127. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bortolami, A.; Williams, N.J.; McGowan, C.M.; Kelly, P.G.; Archer, D.C.; Corrò, M.; Pinchbeck, G.; Saunders, C.J.; Timofte, D. Environmental surveillance identifies multiple introductions of MRSA CC398 in an Equine Veterinary Hospital in the UK, 2011–2016. Sci. Rep. 2017, 7, 5499. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fluit, A. Livestock-associated Staphylococcus aureus. Clin. Microbiol. Infect. 2012, 18, 735–744. [Google Scholar] [CrossRef] [Scilit]
- He, W.; Liu, Y.; Qi, J.; Chen, H.; Zhao, C.; Zhang, F.; Li, H.; Wang, H. Food-animal related Staphylococcus aureus multidrug-resistant ST9 strains with toxin genes. Foodborne Pathog. Dis. 2013, 10, 782–788. [Google Scholar] [CrossRef] [Scilit]
- Taniguchi, Y.; Koide, S.; Maeyama, Y.; Tamai, K.; Hayashi, W.; Tanaka, H.; Iimura, M.; Suzuki, M.; Nagano, Y.; Arakawa, Y. Predominance of methicillin-resistant Staphylococcus aureus SCCmec type II-CC5 and SCCmec type IV-CC1/CC8 among companion animal clinical isolates in Japan: Findings from phylogenetic comparison with human clinical isolates. J. Glob. Antimicrob. Resist. 2020, 20, 253–259. [Google Scholar] [CrossRef] [Scilit]
- Alkuraythi, D.M.; Alkhulaifi, M.M. Methicillin-resistant Staphylococcus aureus prevalence in food-producing animals and food products in Saudi Arabia: A review. Vet. World 2024, 17, 1753. [Google Scholar] [CrossRef] [Scilit]
- Habib, I.; Lakshmi, G.B.; Mohamed, M.-Y.I.; Ghazawi, A.; Khan, M.; Al-Rifai, R.H.; Abdalla, A.; Anes, F.; Elbediwi, M.; Khalifa, H.O. Staphylococcus spp. in salad vegetables: Biodiversity, antimicrobial resistance, and first identification of methicillin-resistant strains in the United Arab Emirates food supply. Foods 2024, 13, 2439. [Google Scholar] [CrossRef] [Scilit]
- Otto, M. MRSA virulence and spread. Cell. Microbiol. 2012, 14, 1513–1521. [Google Scholar] [CrossRef] [Scilit]
- Cheung, G.Y.; Bae, J.S.; Otto, M. Pathogenicity and virulence of Staphylococcus aureus. Virulence 2021, 12, 547–569. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Y.; Xu, D.; Shi, L.; Cai, R.; Li, C.; Yan, H. Association between agr type, virulence factors, biofilm formation and antibiotic resistance of Staphylococcus aureus isolates from pork production. Front. Microbiol. 2018, 9, 1876. [Google Scholar] [CrossRef] [Scilit]
- Jiang, H.; Wang, K.; Yan, M.; Ye, Q.; Lin, X.; Chen, L.; Ye, Y.; Zhang, L.; Liu, J.; Huang, T. Pathogenic and virulence factor detection on viable but non-culturable methicillin-resistant Staphylococcus aureus. Front. Microbiol. 2021, 12, 630053. [Google Scholar] [CrossRef] [Scilit]
- Argudín, M.Á.; Mendoza, M.C.; Rodicio, M.R. Food poisoning and Staphylococcus aureus enterotoxins. Toxins 2010, 2, 1751–1773. [Google Scholar] [CrossRef] [Scilit]
- Hennekinne, J.-A.; De Buyser, M.-L.; Dragacci, S. Staphylococcus aureus and its food poisoning toxins: Characterization and outbreak investigation. FEMS Microbiol. Rev. 2012, 36, 815–836. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mairi, A.; Ibrahim, N.A.; Idres, T.; Touati, A. A Comprehensive review of detection methods for Staphylococcus aureus and its Enterotoxins in Food: From traditional to emerging technologies. Toxins 2025, 17, 319. [Google Scholar] [CrossRef] [Scilit]
- Alghizzi, M.; Shami, A. Staphylococcus aureus as food-borne disease: An ongoing threat in public health in the Kingdom of Saudi Arabia. J. Pure Appl. Microbiol. 2023, 17, 2624–2633. [Google Scholar] [CrossRef] [Scilit]
- Fisher, E.L.; Otto, M.; Cheung, G.Y. Basis of virulence in enterotoxin-mediated staphylococcal food poisoning. Front. Microbiol. 2018, 9, 436. [Google Scholar] [CrossRef] [Scilit]
- Moreno, J.; Diana, L.; Martínez, M.; Iribarnegaray, V.; Puentes, R. Comprehensive analysis of antimicrobial resistance, biofilm formation and virulence factors of staphylococci isolated from bovine mastitis. Heliyon 2025, 11, e42749. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Löffler, B.; Hussain, M.; Grundmeier, M.; Brück, M.; Holzinger, D.; Varga, G.; Roth, J.; Kahl, B.C.; Proctor, R.A.; Peters, G. Staphylococcus aureus panton-valentine leukocidin is a very potent cytotoxic factor for human neutrophils. PLoS Pathog. 2010, 6, e1000715. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shallcross, L.J.; Fragaszy, E.; Johnson, A.M.; Hayward, A.C. The role of the Panton-Valentine leucocidin toxin in staphylococcal disease: A systematic review and meta-analysis. Lancet Infect. Dis. 2013, 13, 43–54. [Google Scholar] [CrossRef] [Scilit]
- Tromp, A.T.; Van Strijp, J.A. Studying staphylococcal leukocidins: A challenging endeavor. Front. Microbiol. 2020, 11, 611. [Google Scholar] [CrossRef] [Scilit]
- Umar, K.; Abdullahi, I.N.; Magashi, A.M.; Kawo, A.H.; Usman, Y.; Ahmad, A.E.-f.; Torres, C. Prevalence and clonal lineages of biofilm-producing Staphylococcus aureus from clinical samples and healthcare workers at Ahmadu Bello University Teaching Hospital, Nigeria. GMS Hyg. Infect. Control 2024, 19, Doc49. [Google Scholar] [PubMed]
- Vittorakis, E.; Vică, M.L.; Zervaki, C.O.; Vittorakis, E.; Maraki, S.; Mavromanolaki, V.E.; Schürger, M.E.; Neculicioiu, V.S.; Papadomanolaki, E.; Sinanis, T. Examining the prevalence and antibiotic susceptibility of S. aureus strains in hospitals: An analysis of the pvl gene and its co-occurrence with other virulence factors. Microorganisms 2023, 11, 841. [Google Scholar] [CrossRef] [Scilit]
- Kaneko, H.; Kanai, M.; Saito, T.; Yanagi, Y.; Kobayashi, H.; Kurihara, R.; Ikeda, M.; Nemoto, O.; Baba, N.; Matsuzaki, Y. Significant increase in the prevalence of Panton–Valentine leukocidin-positive methicillin-resistant Staphylococcus aureus, particularly the USA300 variant ΨUSA300, in the Japanese community. Microbiol. Spectr. 2023, 11, e01248-23. [Google Scholar] [CrossRef] [Scilit]
- Briki, A.; Alkhatib, N.; Aloba, B.; Verma, S.; Nassar, R.; Everett, D.; Ehricht, R.; Monecke, S.; Senok, A. Molecular epidemiology of methicillin-resistant Staphylococcus aureus in Gulf Cooperation Council countries (2010–2025): A scoping review. Front. Microbiol. 2025, 16, 1714252, Correction in Front. Microbiol. 2026, 17, 1791202. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tang, Y.; Li, Y.; Xiao, N.; Wang, L.; Li, S.; Zou, J.; Yu, Y.; Shao, J.; Jiang, M. Antibiotic Resistance, Biofilm Formation, and Molecular Epidemiology of Foodborne Staphylococcus aureus Isolated in Northwest Hubei Province, China. Food Sci. Nutr. 2025, 13, e70791. [Google Scholar] [CrossRef] [Scilit]
- Šmitran, A.; Sladojević, Ž.; Božić, L.; Gajić, I.; Marković, T.; Kasagić, D.; Subić, I.; Katalina, G.; Golić, B. Comparison of biofilm production and virulence genes distribution among human and canine isolates of Staphylococcus aureus. Iran. J. Vet. Res. 2023, 24, 74. [Google Scholar]
- Dandrawy, M.K.; Atiyahullah, T.M.; Saber, H.; Hadad, G.; Abdelaleem, M.M.; Diab, H.M.; Abdelhafeez, H.H.; Ahmed, A.S.; El-Zamkan, M.A.; Elbarbary, N.K. Unleashing the biological potential of marine algal extracts against Staphylococcus aureus isolated from ready-to-eat beef products. Sci. Rep. 2025, 15, 30111. [Google Scholar]
- Foster, T.J.; Höök, M. Surface protein adhesins of Staphylococcus aureus. Trends Microbiol. 1998, 6, 484–488. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Touaitia, R.; Mairi, A.; Ibrahim, N.A.; Basher, N.S.; Idres, T.; Touati, A. Staphylococcus aureus: A review of the pathogenesis and virulence mechanisms. Antibiotics 2025, 14, 470. [Google Scholar] [CrossRef] [Scilit]
- Foster, C.E.; Kok, M.; Flores, A.R.; Minard, C.G.; Luna, R.A.; Lamberth, L.B.; Kaplan, S.L.; Hulten, K.G. Adhesin genes and biofilm formation among pediatric Staphylococcus aureus isolates from implant-associated infections. PLoS ONE 2020, 15, e0235115. [Google Scholar] [CrossRef] [Scilit]
- Ren, Q.; Liao, G.; Wu, Z.; Lv, J.; Chen, W. Prevalence and characterization of Staphylococcus aureus isolates from subclinical bovine mastitis in southern Xinjiang, China. J. Dairy Sci. 2020, 103, 3368–3380. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Soltani, E.; Farrokhi, E.; Zamanzad, B.; Shahini Shams Abadi, M.; Deris, F.; Soltani, A.; Gholipour, A. Prevalence and distribution of adhesins and the expression of fibronectin-binding protein (FnbA and FnbB) among Staphylococcus aureus isolates from Shahrekord Hospitals. BMC Res. Notes 2019, 12, 49. [Google Scholar] [CrossRef] [Scilit]
- Rodríguez-Lázaro, D.; Alonso-Calleja, C.; Oniciuc, E.A.; Capita, R.; Gallego, D.; González-Machado, C.; Wagner, M.; Barbu, V.; Eiros-Bouza, J.M.; Nicolau, A.I. Characterization of biofilms formed by foodborne methicillin-resistant Staphylococcus aureus. Front. Microbiol. 2018, 9, 3004. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vergara, A.; Normanno, G.; Di Ciccio, P.; Pedonese, F.; Nuvoloni, R.; Parisi, A.; Santagada, G.; Colagiorgi, A.; Zanardi, E.; Ghidini, S. Biofilm formation and its relationship with the molecular characteristics of food-related methicillin-resistant Staphylococcus aureus (MRSA). J. Food Sci. 2017, 82, 2364–2370. [Google Scholar] [CrossRef] [Scilit]
- Thiran, E.; Di Ciccio, P.; Graber, H.; Zanardi, E.; Ianieri, A.; Hummerjohann, J. Biofilm formation of Staphylococcus aureus dairy isolates representing different genotypes. J. Dairy Sci. 2018, 101, 1000–1012. [Google Scholar] [CrossRef] [Scilit]
- Bridier, A.; Sanchez-Vizuete, P.; Guilbaud, M.; Piard, J.-C.; Naitali, M.; Briandet, R. Biofilm-associated persistence of food-borne pathogens. Food Microbiol. 2015, 45, 167–178. [Google Scholar] [CrossRef] [Scilit]
- Giaouris, E.; Heir, E.; Hébraud, M.; Chorianopoulos, N.; Langsrud, S.; Møretrø, T.; Habimana, O.; Desvaux, M.; Renier, S.; Nychas, G.-J. Attachment and biofilm formation by foodborne bacteria in meat processing environments: Causes, implications, role of bacterial interactions and control by alternative novel methods. Meat Sci. 2014, 97, 298–309. [Google Scholar] [CrossRef] [Scilit]
- Aires-de-Sousa, M. Methicillin-resistant Staphylococcus aureus among animals: Current overview. Clin. Microbiol. Infect. 2017, 23, 373–380. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qian, J.; Wu, Z.; Zhu, Y.; Liu, C. One Health: A holistic approach for food safety in livestock. Sci. One Health 2022, 1, 100015. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khalifa, H.O.; Abdelhamid, M.A.; Oreiby, A.; Mohamed, M.-Y.I.; Ramadan, H.; Elfadadny, A.; Pack, S.P.; Yoo, H.S.; Habib, I. Fire under the ashes: A descriptive review on the prevalence of methicillin-resistant Staphylococcus aureus in the food supply chain. J. Agric. Food Res. 2025, 19, 101606. [Google Scholar] [CrossRef] [Scilit]
- Petinaki, E.; Spiliopoulou, I. Methicillin-resistant Staphylococcus aureus among companion and food-chain animals: Impact of human contacts. Clin. Microbiol. Infect. 2012, 18, 626–634. [Google Scholar] [CrossRef] [Scilit]
- Crippa, B.L.; Camargo, C.H.; Rall, V.L.M.; Silva, N.C.C. MRSA: The relationship between animal source foods (ASF) and humans–A One Health Concern. Curr. Food Sci. Technol. Rep. 2025, 3, 22. [Google Scholar] [CrossRef] [Scilit]
- Cuny, C.; Wieler, L.H.; Witte, W. Livestock-associated MRSA: The impact on humans. Antibiotics 2015, 4, 521–543. [Google Scholar] [CrossRef] [Scilit]
- Fetsch, A.; Etter, D.; Johler, S. Livestock-associated meticillin-resistant Staphylococcus aureus—Current situation and impact from a One Health perspective. Curr. Clin. Microbiol. Rep. 2021, 8, 103–113. [Google Scholar] [CrossRef] [Scilit]
- Elbehiry, A.; Marzouk, E. Staphylococci in livestock: Molecular epidemiology, antimicrobial resistance, and translational strategies for One Health protection. Vet. Sci. 2025, 12, 757. [Google Scholar] [CrossRef] [Scilit]
- Ferguson, D.D.; Leedom Larson, K.R.; Moritz, E.D.; Smith, T.C. The Environment as a Factor Methicillin-Resistant Staphylococcus aureus Transmission. Rev. Environ. Health 2010, 25, 121–134. [Google Scholar]
- Feld, L.; Bay, H.; Angen, Ø.; Larsen, A.R.; Madsen, A.M. Survival of LA-MRSA in dust from swine farms. Ann. Work Expo. Health 2018, 62, 147–156. [Google Scholar] [CrossRef] [Scilit]
- Agersø, Y.; Vigre, H.; Cavaco, L.; Josefsen, M.H. Comparison of air samples, nasal swabs, ear-skin swabs and environmental dust samples for detection of methicillin-resistant Staphylococcus aureus (MRSA) in pig herds. Epidemiol. Infect. 2014, 142, 1727–1736. [Google Scholar] [CrossRef] [Scilit]
- Kozajda, A.; Jeżak, K.; Kapsa, A. Airborne Staphylococcus aureus in different environments—A review. Environ. Sci. Pollut. Res. 2019, 26, 34741–34753. [Google Scholar] [CrossRef] [Scilit]
- Sergelidis, D.; Angelidis, A.S. Methicillin-resistant Staphylococcus aureus: A controversial food-borne pathogen. Lett. Appl. Microbiol. 2017, 64, 409–418. [Google Scholar] [CrossRef] [Scilit]
- Barua, N.; Rahman, N.; Tin, M.C.; Yang, L.; Alim, A.; Akther, F.; Handapangoda, N.; Manathunga, T.A.; Jinadasa, R.N.; Liyanapathirana, V. Prevalence of MRSA in Livestock, Including Cattle, Farm Animals, and Poultry, in Mainland China, Hong Kong Special Administrative Region, Sri Lanka, and Bangladesh: A Systematic Review and Meta-Analysis. Microorganisms 2025, 13, 704. [Google Scholar] [CrossRef] [Scilit]
- Komodromos, D.; Kotzamanidis, C.; Giantzi, V.; Pappa, S.; Papa, A.; Zdragas, A.; Angelidis, A.; Sergelidis, D. Prevalence, infectious characteristics and genetic diversity of Staphylococcus aureus and methicillin-resistant Staphylococcus aureus (MRSA) in two raw-meat processing establishments in Northern Greece. Pathogens 2022, 11, 1370. [Google Scholar]
- Mohammed, R.; Nader, S.M.; Hamza, D.A.; Sabry, M.A. Public health implications of multidrug-resistant and methicillin-resistant Staphylococcus aureus in retail oysters. Sci. Rep. 2025, 15, 4496. [Google Scholar] [CrossRef] [Scilit]
- Ala’a, B.; Momani, S.; Hasan, H.; Obeidat, A.; Horabi, M. Tackling antimicrobial resistance in the food chain under the One Health umbrella: A systems thinking approach with a focus on Jordan. Sci. One Health 2025, 4, 100115. [Google Scholar]
- Islam, M.A.; Bose, P.; Rahman, M.Z.; Muktaruzzaman, M.; Sultana, P.; Ahamed, T.; Khatun, M.M. A review of antimicrobial usage practice in livestock and poultry production and its consequences on human and animal health. J. Adv. Vet. Anim. Res. 2024, 11, 675. [Google Scholar] [CrossRef] [Scilit]
- Aenishaenslin, C.; Häsler, B.; Ravel, A.; Parmley, E.J.; Mediouni, S.; Bennani, H.; Stärk, K.D.; Buckeridge, D.L. Evaluating the integration of one health in surveillance systems for antimicrobial use and resistance: A conceptual framework. Front. Vet. Sci. 2021, 8, 611931. [Google Scholar]
- Bordier, M.; Uea-Anuwong, T.; Binot, A.; Hendrikx, P.; Goutard, F.L. Characteristics of One Health surveillance systems: A systematic literature review. Prev. Vet. Med. 2020, 181, 104560. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sudatip, D.; Tiengrim, S.; Chasiri, K.; Kritiyakan, A.; Phanprasit, W.; Morand, S.; Thamlikitkul, V. One health surveillance of antimicrobial resistance phenotypes in selected communities in Thailand. Antibiotics 2022, 11, 556. [Google Scholar] [CrossRef] [Scilit]
- Delpy, L.; Astbury, C.C.; Aenishaenslin, C.; Ruckert, A.; Penney, T.L.; Wiktorowicz, M.; Ciss, M.; Benko, R.; Bordier, M. Integrated surveillance systems for antibiotic resistance in a One Health context: A scoping review. BMC Public Health 2024, 24, 1717. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lloyd, D.H.; Page, S.W. Antimicrobial stewardship in veterinary medicine. In Antimicrobial Resistance in Bacteria from Livestock and Companion Animals; Schwarz, S., Cavaco, L.M., Shen, J., Eds.; ASM Press: Washington, DC, USA, 2018; pp. 507–524. [Google Scholar] [CrossRef] [Scilit]
- Gomes, E.; Mesquita, T.G.; Serra, P.; Araújo, D.; Almeida, C.; Machado, A.; Oliveira, R.; Castro, J. Antimicrobial Resistance in the Food Chain: Bridging Knowledge Gaps for Effective Detection and Control. Antibiotics 2026, 15, 262. [Google Scholar] [CrossRef] [Scilit]
- Arama, U.O.; Oduoye, M.O.; Akanbi-Hakeem, B.; Khan, M.; Wechuli, P.; Aliyu, A. A systematic review of One Health perspective on the use of antimicrobials in Nigeria. CABI One Health 2025, 4, 0004. [Google Scholar] [CrossRef] [Scilit]
- Sawodny, S.; Käsbohrer, A.; Bröker, L.; Firth, C.; Marschik, T. Intervention strategies for methicillin-resistant Staphylococcus aureus control in pig farming: A comprehensive review. Porc. Health Manag. 2025, 11, 17. [Google Scholar]
- Islam, M.S.; Wollie, A.M.; Razu, S.; Gebeyehu, D.T.; Jahan, N.; Kasse, G.E. Antimicrobial resistance in food-related sources: A One Health perspective through comparative meta-analysis. Crit. Public Health 2026, 36, 2607343. [Google Scholar]
- Alarawi, M.S.; Altammami, M.; Abutarboush, M.; Kulmanov, M.; Alkuraithy, D.M.; Kafkas, S.; Radley, R.; Abdelhakim, M.; Aldakhil, H.; Bawazeer, R.A. Genomic diversity and antimicrobial resistance of Staphylococcus aureus in Saudi Arabia: A nationwide study using whole-genome sequencing. Microb. Genom. 2025, 11, 001540. [Google Scholar] [CrossRef] [Scilit]
- Pennone, V.; Cobo-Díaz, J.F.; Prieto, M.; Alvarez-Ordóñez, A. Application of genomics and metagenomics to improve food safety based on an enhanced characterisation of antimicrobial resistance. Curr. Opin. Food Sci. 2022, 43, 183–188. [Google Scholar] [CrossRef] [Scilit]
- Chigozie, V.U.; Aniokete, C.U.; Ogbonna, P.I.; Iroha, R.I. Transforming antimicrobial resistance mitigation: The genomic revolution in one health and public health. Discov. Appl. Sci. 2025, 7, 1187. [Google Scholar] [CrossRef] [Scilit]
- Djordjevic, S.P.; Jarocki, V.M.; Seemann, T.; Cummins, M.L.; Watt, A.E.; Drigo, B.; Wyrsch, E.R.; Reid, C.J.; Donner, E.; Howden, B.P. Genomic surveillance for antimicrobial resistance—A One Health perspective. Nat. Rev. Genet. 2024, 25, 142–157. [Google Scholar] [CrossRef] [Scilit]
- Tiwari, S.; Dhakal, T.; Kim, B.-J.; Jang, G.S.; Oh, Y. Genomics in epidemiology and disease surveillance: An exploratory analysis. Life 2025, 15, 1848. [Google Scholar] [CrossRef] [Scilit] [PubMed]


| Antibiotic Class | Major Resistance Genes | Mechanism of Resistance | References |
|---|---|---|---|
| Macrolides/Lincosamides | ermA, ermB, ermC | Ribosomal methylation of 23S rRNA preventing binding of MLSB antibiotics | [84,85] |
| Macrolides/Streptogramins | msrA | ATP-binding cassette efflux transporter exporting macrolides | [85] |
| Tetracyclines | tetK | Membrane efflux pump reducing intracellular tetracycline concentration | [86] |
| tetM | Ribosomal protection protein displacing tetracycline from the ribosome | [86] | |
| Fluoroquinolones | gyrA/gyrB mutations | Target modification of DNA gyrase | [87] |
| grlA/grlB mutations | Target modification of topoisomerase IV | [87] | |
| Multidrug resistance | norA | Major facilitator superfamily (MFS) efflux pump exporting multiple antibiotics | [72] |
| norB, norC | Multidrug efflux transporters contributing to drug efflux | [72] | |
| mepA | MATE family multidrug efflux pump | [88] | |
| Antiseptics/disinfectants | qacA, qacB | Plasmid-encoded efflux pumps conferring tolerance to quaternary ammonium compounds | [81,82] |
| Food Product | Country/Region | Main Finding | Reference |
|---|---|---|---|
| Animal-derived foods | Italy | MRSA detected in 0.37% (6/1634) | [103] |
| Retail meat | Netherlands | MRSA detected in 11.9% (264/2217) | [99] |
| United States | MRSA detected in 6.6% (9/136) | [100] | |
| MRSA detected in 1.2% (2/165) | [104] | ||
| Retail meat (isolates) | China | MRSA detected in 7.4% of S. aureus isolates (48/648) | [101] |
| Retail foods | MRSA detected in 2.5% (5/197) | [105] | |
| Raw milk & dairy | Iran | MRSA detected in ~2.0% (53/2650) | [106] |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.
Share and Cite
Elbehiry, A.; Abalkhail, A.; Elmanssury, A.E.; Marzouk, E. Methicillin-Resistant Staphylococcus aureus in the Food Chain: Molecular Epidemiology, Resistance Mechanisms, and Public Health Implications. Int. J. Mol. Sci. 2026, 27, 3814. https://doi.org/10.3390/ijms27093814
Elbehiry A, Abalkhail A, Elmanssury AE, Marzouk E. Methicillin-Resistant Staphylococcus aureus in the Food Chain: Molecular Epidemiology, Resistance Mechanisms, and Public Health Implications. International Journal of Molecular Sciences. 2026; 27(9):3814. https://doi.org/10.3390/ijms27093814
Chicago/Turabian StyleElbehiry, Ayman, Adil Abalkhail, Ahmed Elnadif Elmanssury, and Eman Marzouk. 2026. "Methicillin-Resistant Staphylococcus aureus in the Food Chain: Molecular Epidemiology, Resistance Mechanisms, and Public Health Implications" International Journal of Molecular Sciences 27, no. 9: 3814. https://doi.org/10.3390/ijms27093814
APA StyleElbehiry, A., Abalkhail, A., Elmanssury, A. E., & Marzouk, E. (2026). Methicillin-Resistant Staphylococcus aureus in the Food Chain: Molecular Epidemiology, Resistance Mechanisms, and Public Health Implications. International Journal of Molecular Sciences, 27(9), 3814. https://doi.org/10.3390/ijms27093814