Article

Competition-Induced Neuroendocrine–Immune Crosstalk in Elite Water Polo Players: Salivary Cytokine, Cortisol, and IgA Dynamics


1
Istituto di Ricovero e Cura a Carattere Scientifico ‘G. Gaslini’ Institute, 16147 Genova, Italy
2
Department of Neurosciences, Rehabilitation, Ophthalmology, Genetics, Maternal and Child Health, University of Genoa, 16132 Genova, Italy
3
Dipartimento di Storia Culture Civiltà, University of Bologna, 40124 Bologna, Italy
4
Department of Experimental Medicine, University of Genoa, 16132 Genova, Italy
5
Laboratory Medicine, Istituto di Ricovero e Cura a Carattere Scientifico Azienda Ospedaliera Metropolitana, Plesso San Martino, 16132 Genova, Italy
6
Diagnostic Autoimmunology Laboratory, Istituto di Ricovero e Cura a Carattere Scientifico Azienda Ospedaliera Metropolitana, Plesso San Martino, 16132 Genova, Italy
*
Author to whom correspondence should be addressed.
These authors contributed equally to this work.
BioChem 2026, 6(3), 16; https://doi.org/10.3390/biochem6030016
Submission received: 6 May 2026 / Revised: 18 June 2026 / Accepted: 24 June 2026 / Published: 26 June 2026

Abstract

Background: Competitive sports represent a powerful physiological and psychological stressor capable of modulating neuroendocrine and immune pathways. Water polo, characterized by intense intermittent exertion and frequent physical contact, provides a unique model to investigate competition-related stress biology. Methods: Sixteen male Italian Serie C water polo players were enrolled in the study. Using a within-subject design, saliva samples were collected under controlled circadian conditions. Salivary biomarkers, including cortisol, IgA, and cytokines, were assessed both before and after training sessions and competitive matches. Results: Both training and competition elicited POST-session increases in salivary cortisol and cytokines, alongside reductions in IgA. However, competition produced significantly higher anticipatory and POST-session cortisol concentrations. A larger POST-session decreases in IgA compared with training was observed. Cytokine concentrations increased from PRE- to POST-session in both conditions, with significantly greater induction during competition across the panel. During training, selected cytokines showed positive within-session correlations with cortisol, indicating coordinated hypothalamic–pituitary–adrenal–immune activation under lower psychosocial load. These associations were attenuated and less consistent during competition. Conclusions: Official competition amplifies endocrine and immune responses beyond those observed during match-like training in elite water polo players, despite comparable physical demands. Altered cytokine–cortisol coupling under competitive conditions suggests modulation of neuroendocrine–immune integration by psychosocial stress. Combined salivary profiling of cortisol, cytokines, and IgA represents a feasible, non-invasive approach for monitoring psychophysiological load in elite aquatic team sports.

1. Introduction

Water polo is among the most physiologically and psychologically demanding team sports. Match play requires repeated bouts of high-intensity swimming, rapid accelerations, grappling, and sustained tactical engagement, resulting in substantial metabolic, mechanical, and neuroendocrine load. The intermittent nature of exertion, coupled with frequent physical contact and limited recovery intervals, places water polo athletes under pronounced cardiovascular and musculoskeletal stress [1,2]. However, the demands of competition extend beyond physical exertion alone. Official matches uniquely expose athletes to anticipatory anxiety, social-evaluative stress, and outcome uncertainty, factors that are largely attenuated or absent during routine training sessions [3,4].
Psychological stressors associated with competition are known to activate the hypothalamic–pituitary–adrenal (HPA) axis, leading to elevations in circulating and salivary cortisol [5,6]. Cortisol plays a central role in coordinating energy availability and modulating immune responses, exerting context-dependent effects on inflammation and host defense [7,8]. In athletes, acute increases in cortisol during competition have been repeatedly linked to transient immune perturbations, including alterations in mucosal immunity and cytokine signaling [9,10,11]. Importantly, the magnitude of these responses appears to depend not only on exercise intensity but also on the psychosocial context in which exertion occurs [3,4,11].
Cytokines occupy a central position in this stress–immune interface. Acting as pleiotropic signaling molecules, cytokines orchestrate exercise-induced inflammation, regulate leukocyte trafficking, and contribute to tissue repair and metabolic adaptation following exertion [12,13]. Both pro- and anti-inflammatory cytokines are rapidly mobilized in response to acute exercise, with patterns that depend on intensity, duration, training status, and recovery dynamics [14,15,16]. While these processes have been extensively studied in endurance and resistance exercise paradigms, cytokine responses in water polo remain comparatively underexplored. Direct comparisons between training and competition, and the extent to which cytokine fluctuations are temporally coupled to cortisol within the same session, remain poorly defined.
Understanding these interactions is relevant not only for exercise immunology but also for athlete health and performance management. Dysregulated or repeatedly exaggerated inflammatory responses may impair recovery, increase susceptibility to illness, and contribute to maladaptation across a competitive season [17,18,19,20]. Conversely, tightly coordinated cytokine–cortisol responses may reflect an efficient and resilient stress-adaptation system [21,22].
The present study aimed to systematically compare cytokine and cortisol responses in elite water polo players across matched training and competition sessions. Additionally, we examined within-session relationships between cytokines and cortisol to better characterize neuroendocrine–immune coupling under differing psychosocial demands.
Based on existing evidence [3,4,9,11,17], we preregistered the following directional hypotheses: (1) competitive matches would elicit larger PRE- to POST-session increases in both cytokines and cortisol compared with training sessions; and (2) cytokine concentrations would show positive within-session correlations with cortisol, reflecting coordinated activation of the HPA axis and immune signaling pathways [23].
By addressing these questions, this study seeks to refine current understanding of stress biology in elite team sports and to delineate the distinct immunoendocrine signatures of competition versus training in water polo athletes.

2. Materials and Methods

2.1. Participants and Study Design

The study sample consisted of male water polo players competing in the Italian Serie C league, which represents the third division and a sub-elite level of competition. All participants were members of the same team and adhered to a uniform training regimen that included 4–5 sessions per week (approximately 8–10 h weekly) throughout a competitive season lasting about 8–9 months. Although every athlete took part in all matches, variations in individual playing time and positional responsibilities were not controlled and may have affected physiological outcomes. Players were asked to maintain their usual hydration and dietary practices; however, sleep, nutrition, and supplement intake were not strictly regulated, which should be taken into account when evaluating biomarker variability.
Eligibility required consistent participation in training, while exclusion criteria included recent illness, injury, or the use of medications influencing immune or endocrine function. Health status was assessed via a self-reported questionnaire (see Supplementary Table S1).
A total of sixteen players were included: 2 goalkeepers, 10 field players, and 4 center forwards. The mean age was 23 ± 4 years, with a range of 19 to 27 years.
To control for circadian variation in salivary biomarkers, both sessions were scheduled in the evening. Saliva samples were collected at two time points for each session: PRE, defined as 15–20 min before the start of the session, and POST, defined as 15–20 min after session completion. The study design, sampling timeline, and handling procedures were consistent with those adopted in the cohort’s previously published biomarker investigations, allowing direct comparability across studies.
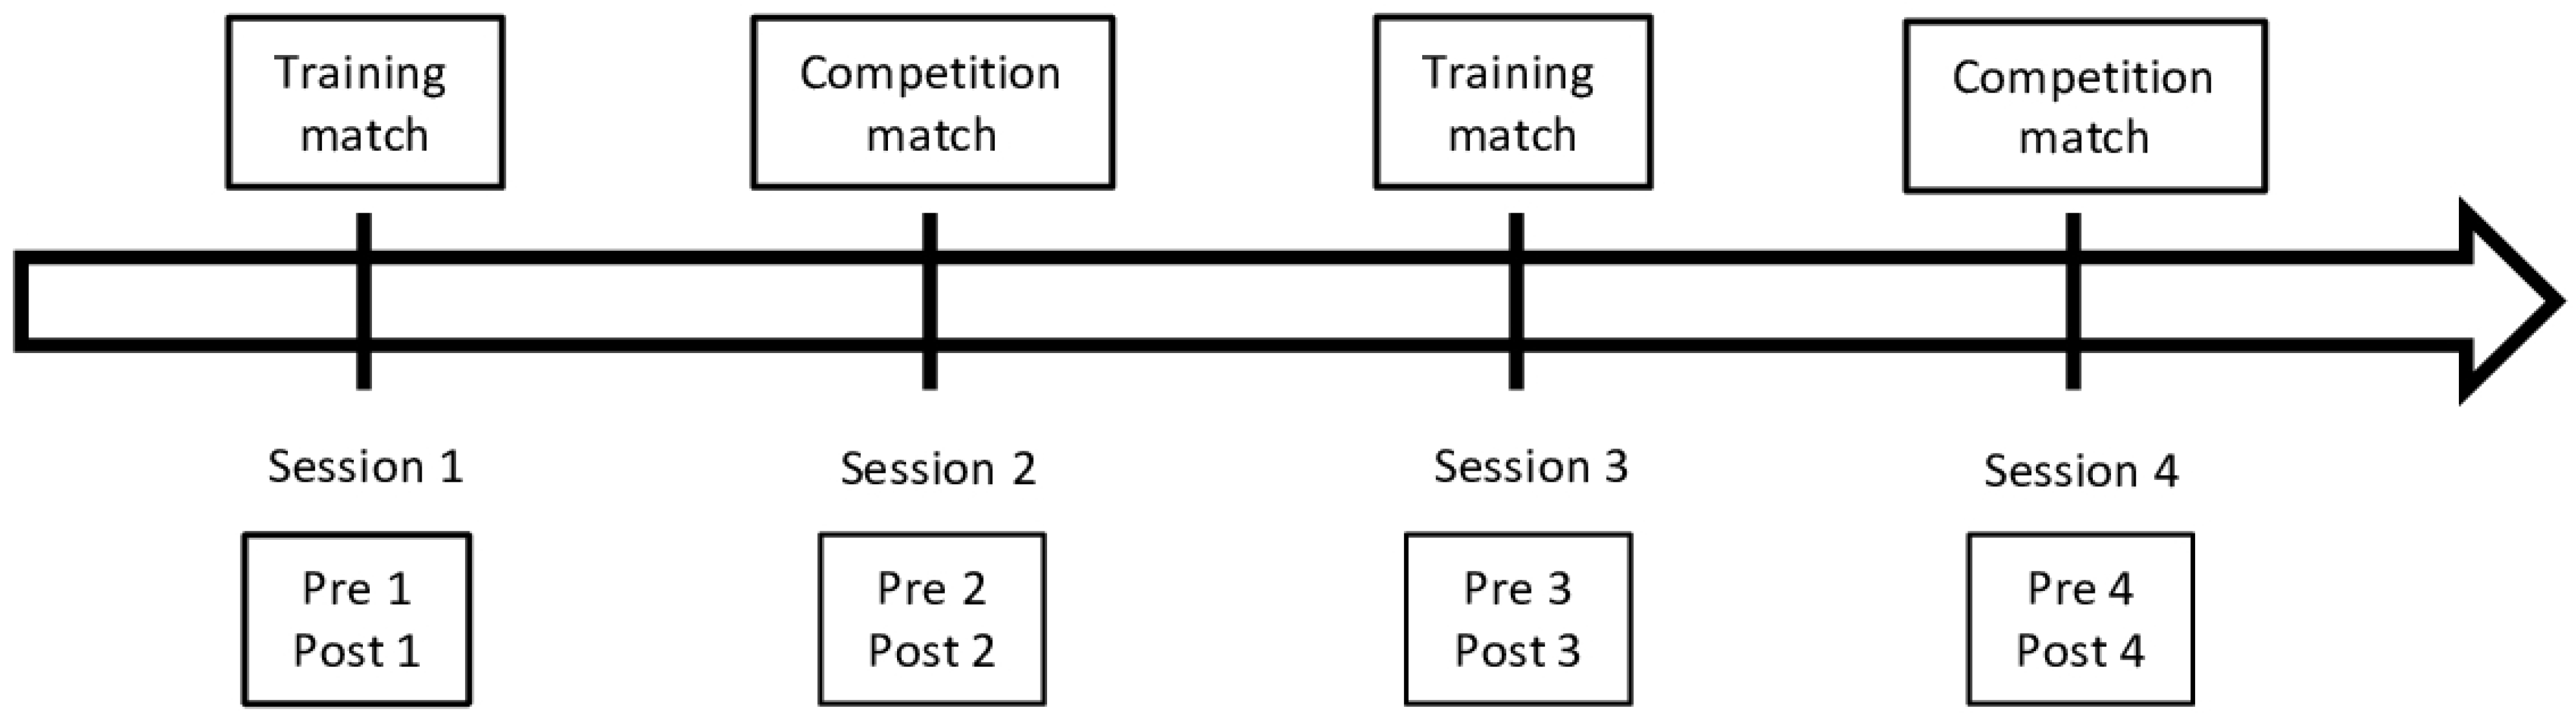
Study design and sampling timeline are shown in Figure 1.
All participants provided written informed consent prior to inclusion, and the study was conducted in accordance with the Declaration of Helsinki and local ethical approval (Ethical Committee of the University of Genoa, CERA 2024/34, 25 March 2024).

2.2. Saliva Collection and Processing

Saliva samples were obtained using commercially available swab-based collection systems validated for field and poolside use (SARSTEDT S.r.l., Trezzano sul Naviglio, Milano, Italy). Participants were instructed to refrain from eating, drinking (except water), brushing teeth, or using oral products for at least 60 min prior to sampling. The absence of blood contamination was checked with a salivary blood contamination kit (Salimetrics LLC, Cambridge, UK).
Following collection, samples were refrigerated during transport, then centrifuged to remove debris, and stored at −80 °C until analysis. All samples were assayed in batches to minimize inter-assay variability, and samples from the same participant were always analyzed within the same assay run.

2.3. Biomarker Assays

Salivary cortisol concentrations were quantified using a high-sensitivity enzyme immunoassay (EIA test, Pantex, Santa Monica, CA, USA), following the manufacturer’s instructions and established laboratory protocols previously applied in this cohort. The assay range was 0.1–30 ng/mL, and the sensitivity 0.0392 ng/mL.
Salivary testosterone and immunoglobulin A (IgA)were measured using enzyme-linked immunosorbent assays (ELISA, by EMELCA Bioscience, Breda, The Netherlands) validated for salivary matrices. The range was 0.2–80 ng/mL, and the sensitivity was <0.1 ng/mL for testosterone. The range was 0.24–1000 ng/mL, and the sensitivity was <0.24 ng/mL for IgA. All samples were tested in triplicate. Intra-assay deviation was 6.3% for the EIA test and <10% for all ELISA kits.
Salivary cytokines were quantified using ELISA-based immunoassays validated for low-volume salivary samples. The cytokine panel comprised key pro-inflammatory mediators relevant to exercise-induced immune modulation. All assays were performed in accordance with the manufacturers’ recommendations (ImmunoTools GmbH, Friesoythe, Germany). The minimum detectable concentrations were 18 pg/mL for IL-1β, 6.1 pg/mL for IL-6, and 22 pg/mL for TNF-α, as reported by the manufacturer. The experiments were repeated three times, and the means ± standard deviations (SDs) were presented. For all the ELISA kits, the intra-assay precision was <8%, and the inter-assay precision was <10%.
The analytical methods were performed using commercially available assay kits validated for salivary samples according to the manufacturer’s specifications. Assay performance characteristics, including sensitivity, intra- and inter-assay variability, and standard curve ranges, were verified prior to analysis. Finally, sample stability was ensured by immediate storage at −20 °C/−80 °C following collection and avoidance of repeated freeze–thaw cycles. Additionally, it was verified that a freeze–thaw cycle, applied to all saliva samples, did not affect the values of the biomarkers analyzed in this study.

2.4. Outcomes

The primary outcomes of the study were the pre- to post-session (PRE → POST) changes in salivary cytokines and cortisol, and the comparison of these responses between training and competition sessions.
Secondary outcomes included within-session associations between cytokine concentrations and cortisol levels, examined separately for training and competition, to explore neuroendocrine–immune coupling under differing psychosocial conditions.

2.5. Statistical Analysis

Statistical analyses for cortisol, testosterone, and IgA followed the repeated-measures analytical framework established in previous studies of this cohort [24]. For cytokine outcomes, data were analyzed using a two-way repeated-measures analysis of variance (ANOVA) with SESSION (training vs. competition) and TIME (PRE vs. POST) as within-subject factors.
Associations between cytokines and cortisol within each session were assessed using Spearman’s rank correlation coefficient, with corresponding 95% confidence intervals.
Statistical analyses were performed using Prism10 (GraphPad Software, Boston, MA, USA).
p values lower than 0.05 were considered as significant.

3. Results

3.1. Cortisol, Testosterone, and IgA: Contextual Markers of Psychophysiological Load

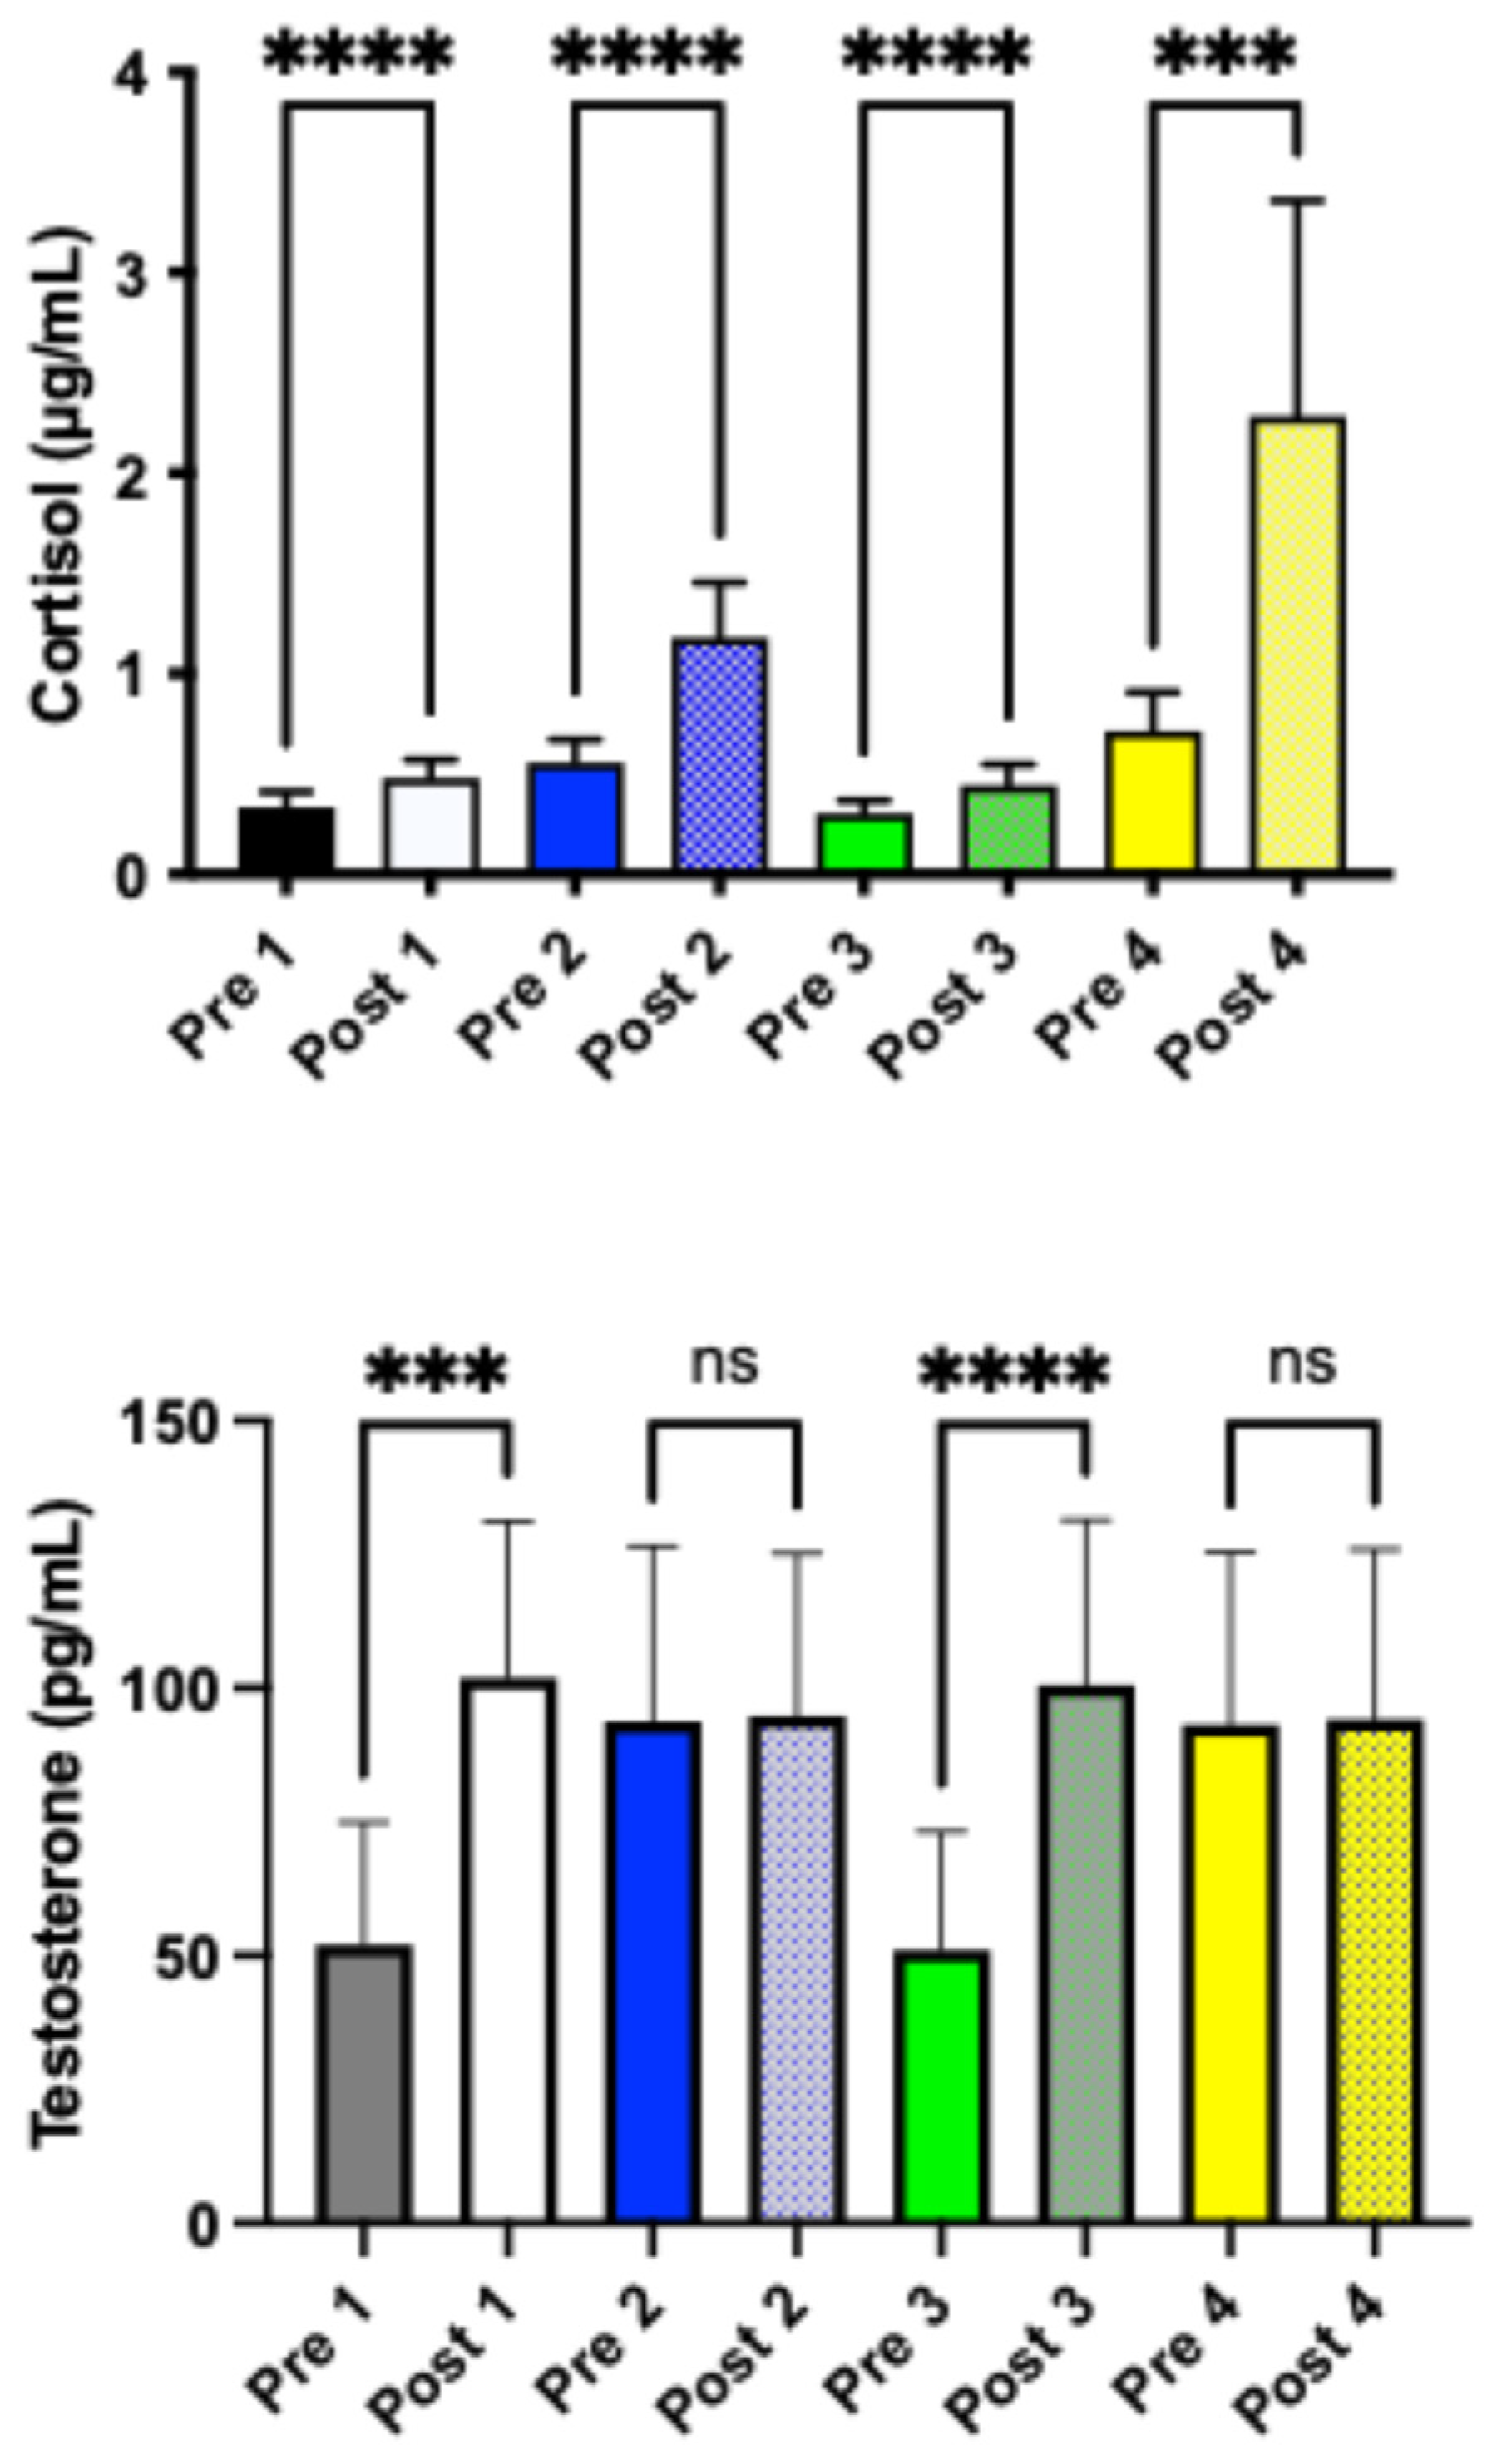
Salivary cortisol concentrations increased significantly from PRE to POST across both experimental conditions, indicating robust activation of the HPA axis in response to water polo activity (main effect of time, p < 0.001). A significant main effect of SESSION was also observed, with higher overall cortisol concentrations during competition compared with training (p < 0.01). All of these results are summarized in Figure 2 (upper box).
Importantly, a significant SESSION × TIME interaction was detected for cortisol (F14,98 = 1.61, p = 0.091), indicating that the magnitude of the PRE → POST cortisol response differed between conditions. Cortisol production significantly PRE → POST increases during both training (p < 0.001) and competition (p < 0.001), with a substantially larger increase during competition. In addition, anticipatory (PRE) cortisol concentrations were significantly higher before competition than before training (p < 0.001).
A significant increase in testosterone concentration was observed following training matches: mean pre-training match (P1) values were markedly higher than post-training match levels (P2): F1,14 = 68.07, p < 0.001. Similarly, a significant pre- (P3) to post- training match (P4) elevation in testosterone (F1,14 = 67.82, p < 0.001).
In contrast, no significant differences were detected between pre- and post-competitive match values: P3 vs. P4 (F1,14 = 0.015, p = 0.91) and P5 vs. P6 (F1,14 = 0.015, p = 0.91), indicating an absence of acute hormonal response in these sessions.
Overall, the results indicate a variable testosterone response across matches, with significant acute increases occurring in training matches, while competitive matches did not elicit significant changes.
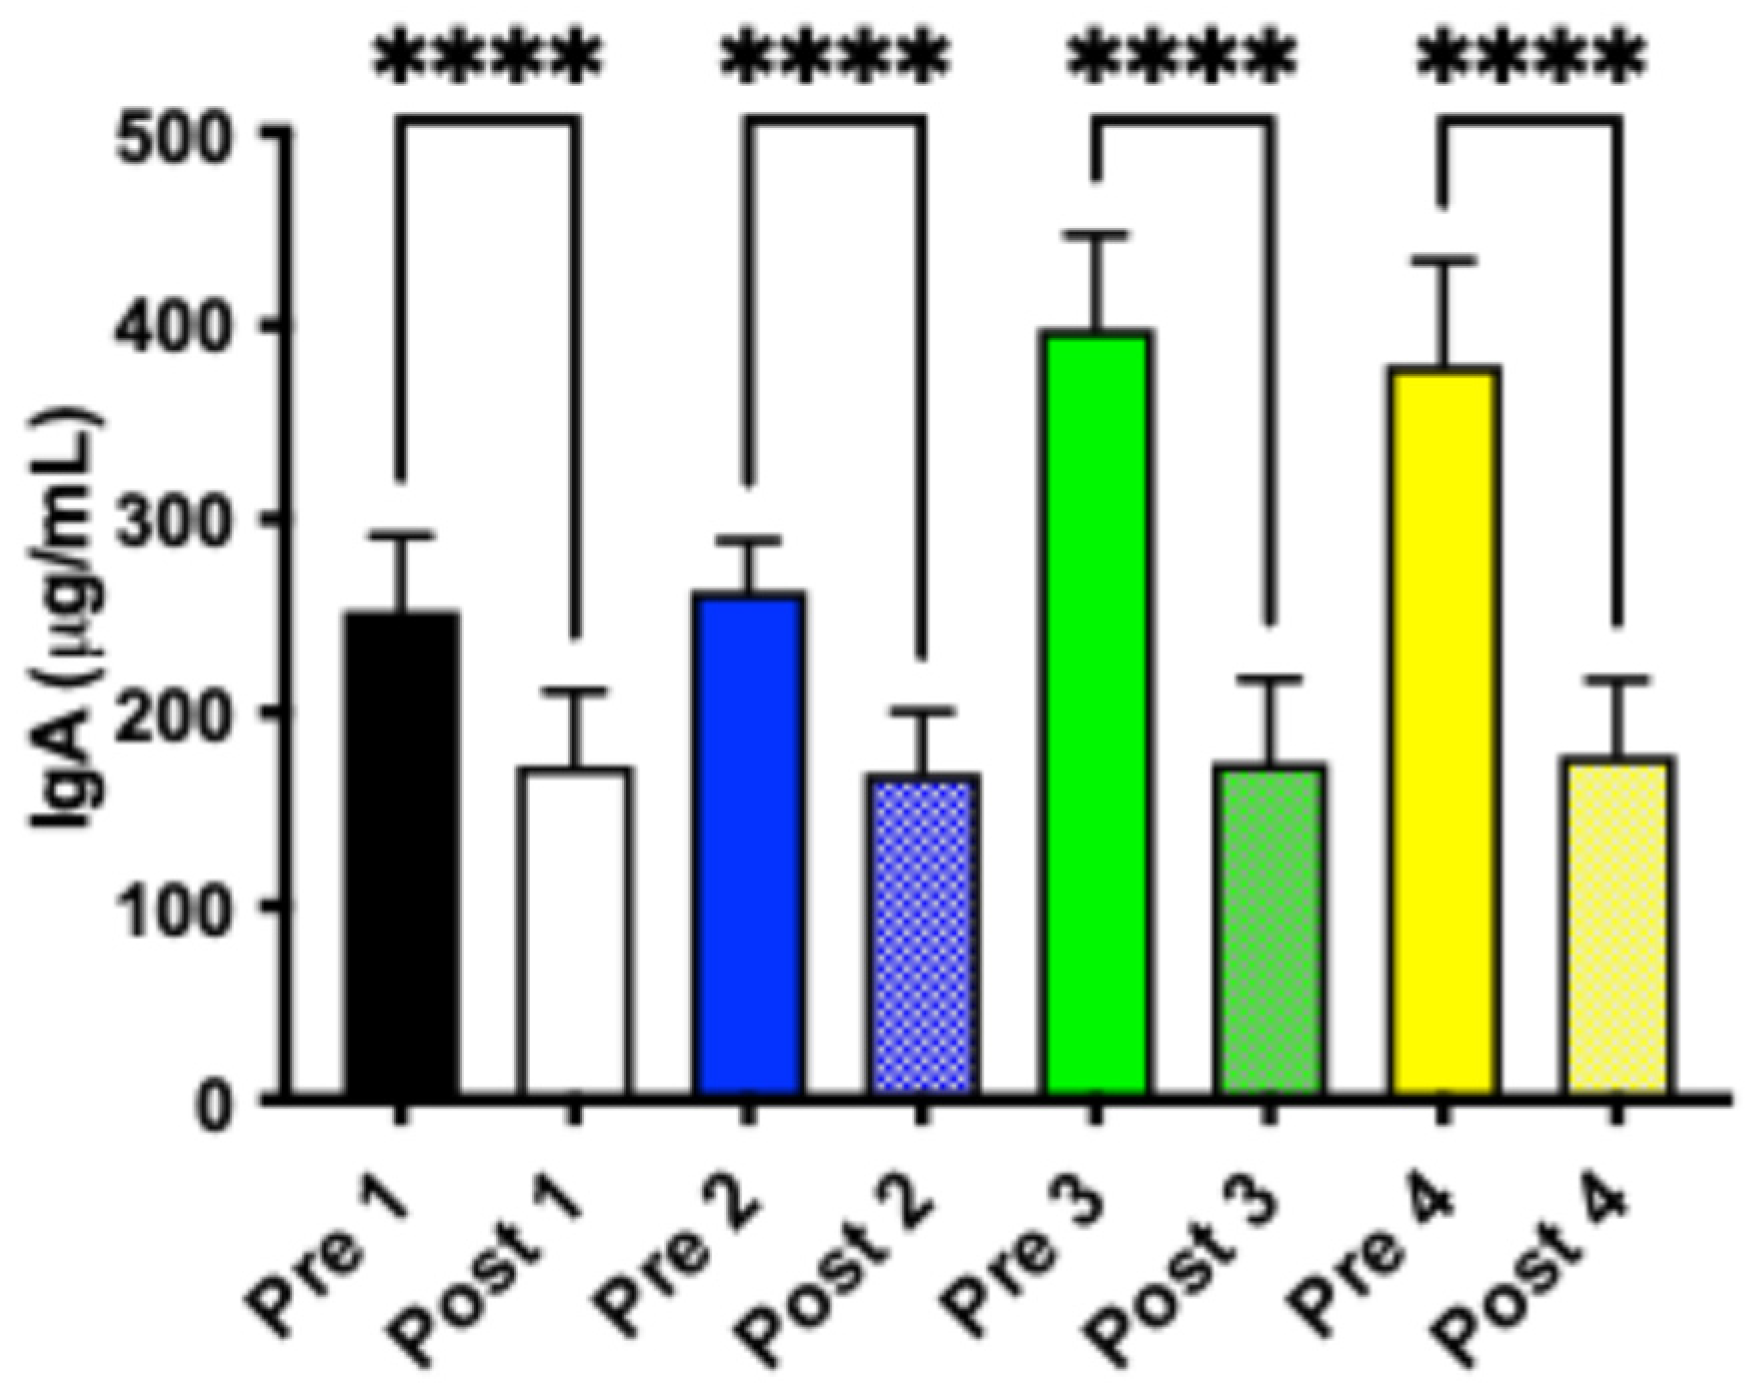
Salivary IgA concentrations decreased significantly from PRE to POST in both conditions (main effect of time, p < 0.001). A significant SESSION × TIME interaction was also observed for IgA (F14,98 = 2.89, p = 0.010). In addition, POST-session reduction in IgA was significantly greater following competition than training (p < 0.001), indicating amplified suppression of mucosal immunity under competitive conditions.
Descriptive statistics for cortisol, testosterone and IgA across sessions and time points are reported in Table 1 and summarized in Figure 2.

3.2. Cytokine Responses Differ Between Training and Competition

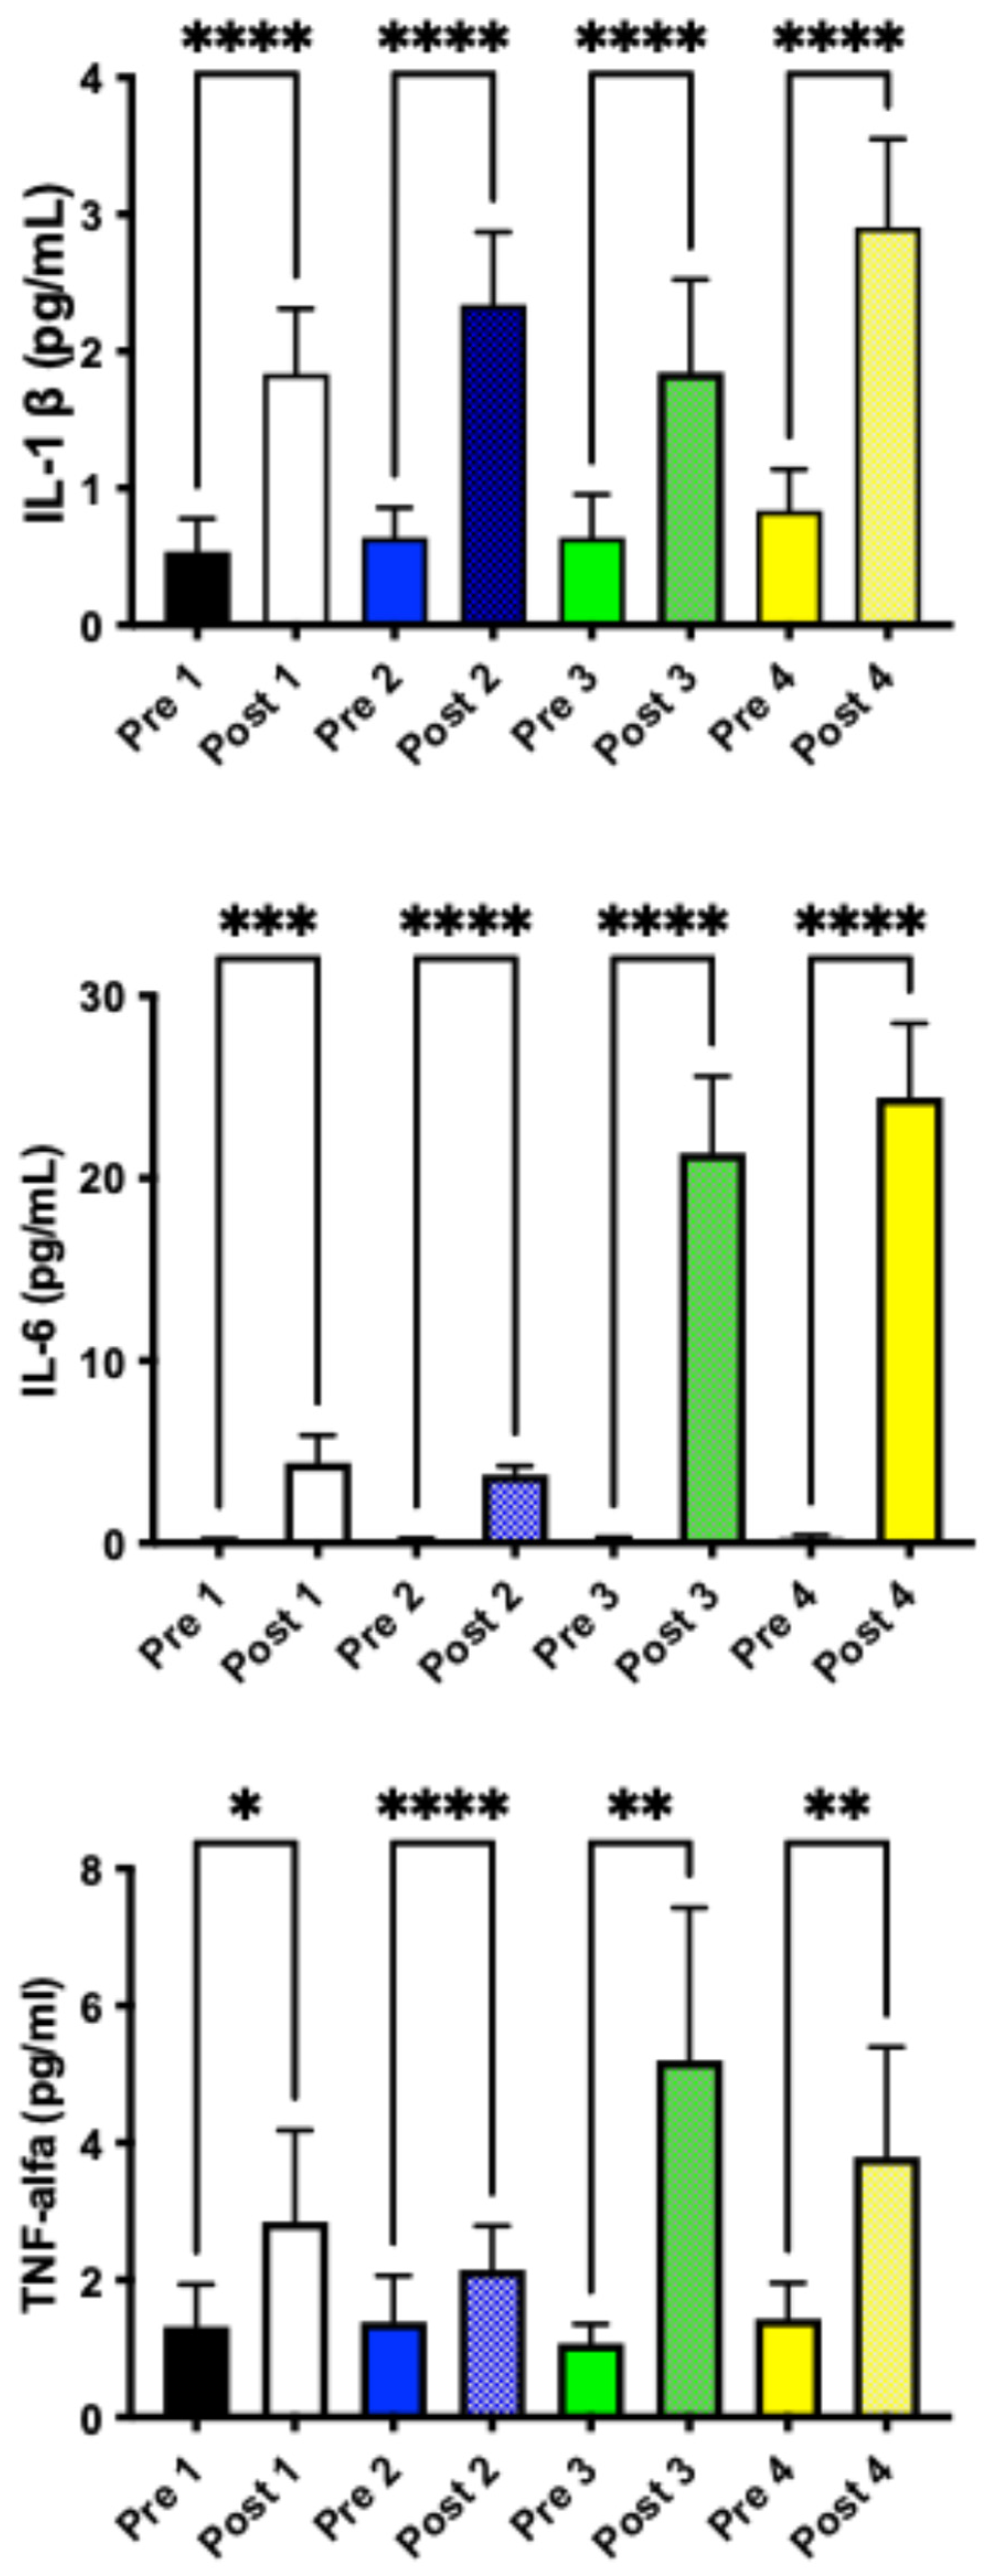
Salivary cytokine concentrations increased from PRE to POST in both training and competition sessions, consistent with activation of exercise-related inflammatory signaling. Two-way repeated-measures ANOVA revealed a significant main effect of TIME for all cytokines examined (p < 0.001), confirming acute post-exercise induction.
A significant main effect of SESSION was observed for multiple cytokines, with higher overall concentrations during competition compared with training (p < 0.001). Crucially, significant SESSION × TIME interactions were detected across the cytokine panel (all p < 0.001), indicating that the magnitude of the PRE → POST cytokine response was modulated by competitive context.
In addition, a PRE → POST increase during competition for all measured cytokines (all p < 0.001) was observed, whereas training-induced changes were smaller and, for some markers, more variable. Among pro-inflammatory mediators, IL-6 exhibited particularly pronounced sensitivity to competition, with significantly greater POST concentrations and fold changes compared with training (p < 0.001). Similar patterns were observed for IL-1β and TNF-α, supporting the presence of an amplified inflammatory response under competitive conditions.
Anti-inflammatory cytokines, where assessed, showed concurrent POST increases, suggesting coordinated immune activation rather than a purely pro-inflammatory shift. Cytokine descriptive statistics and PRE → POST percentage changes are presented in Table 2, while inferential statistics, effect sizes, and interaction terms are summarized in Figure 3.

3.3. Cortisol-Testosterone Coupling Within Section

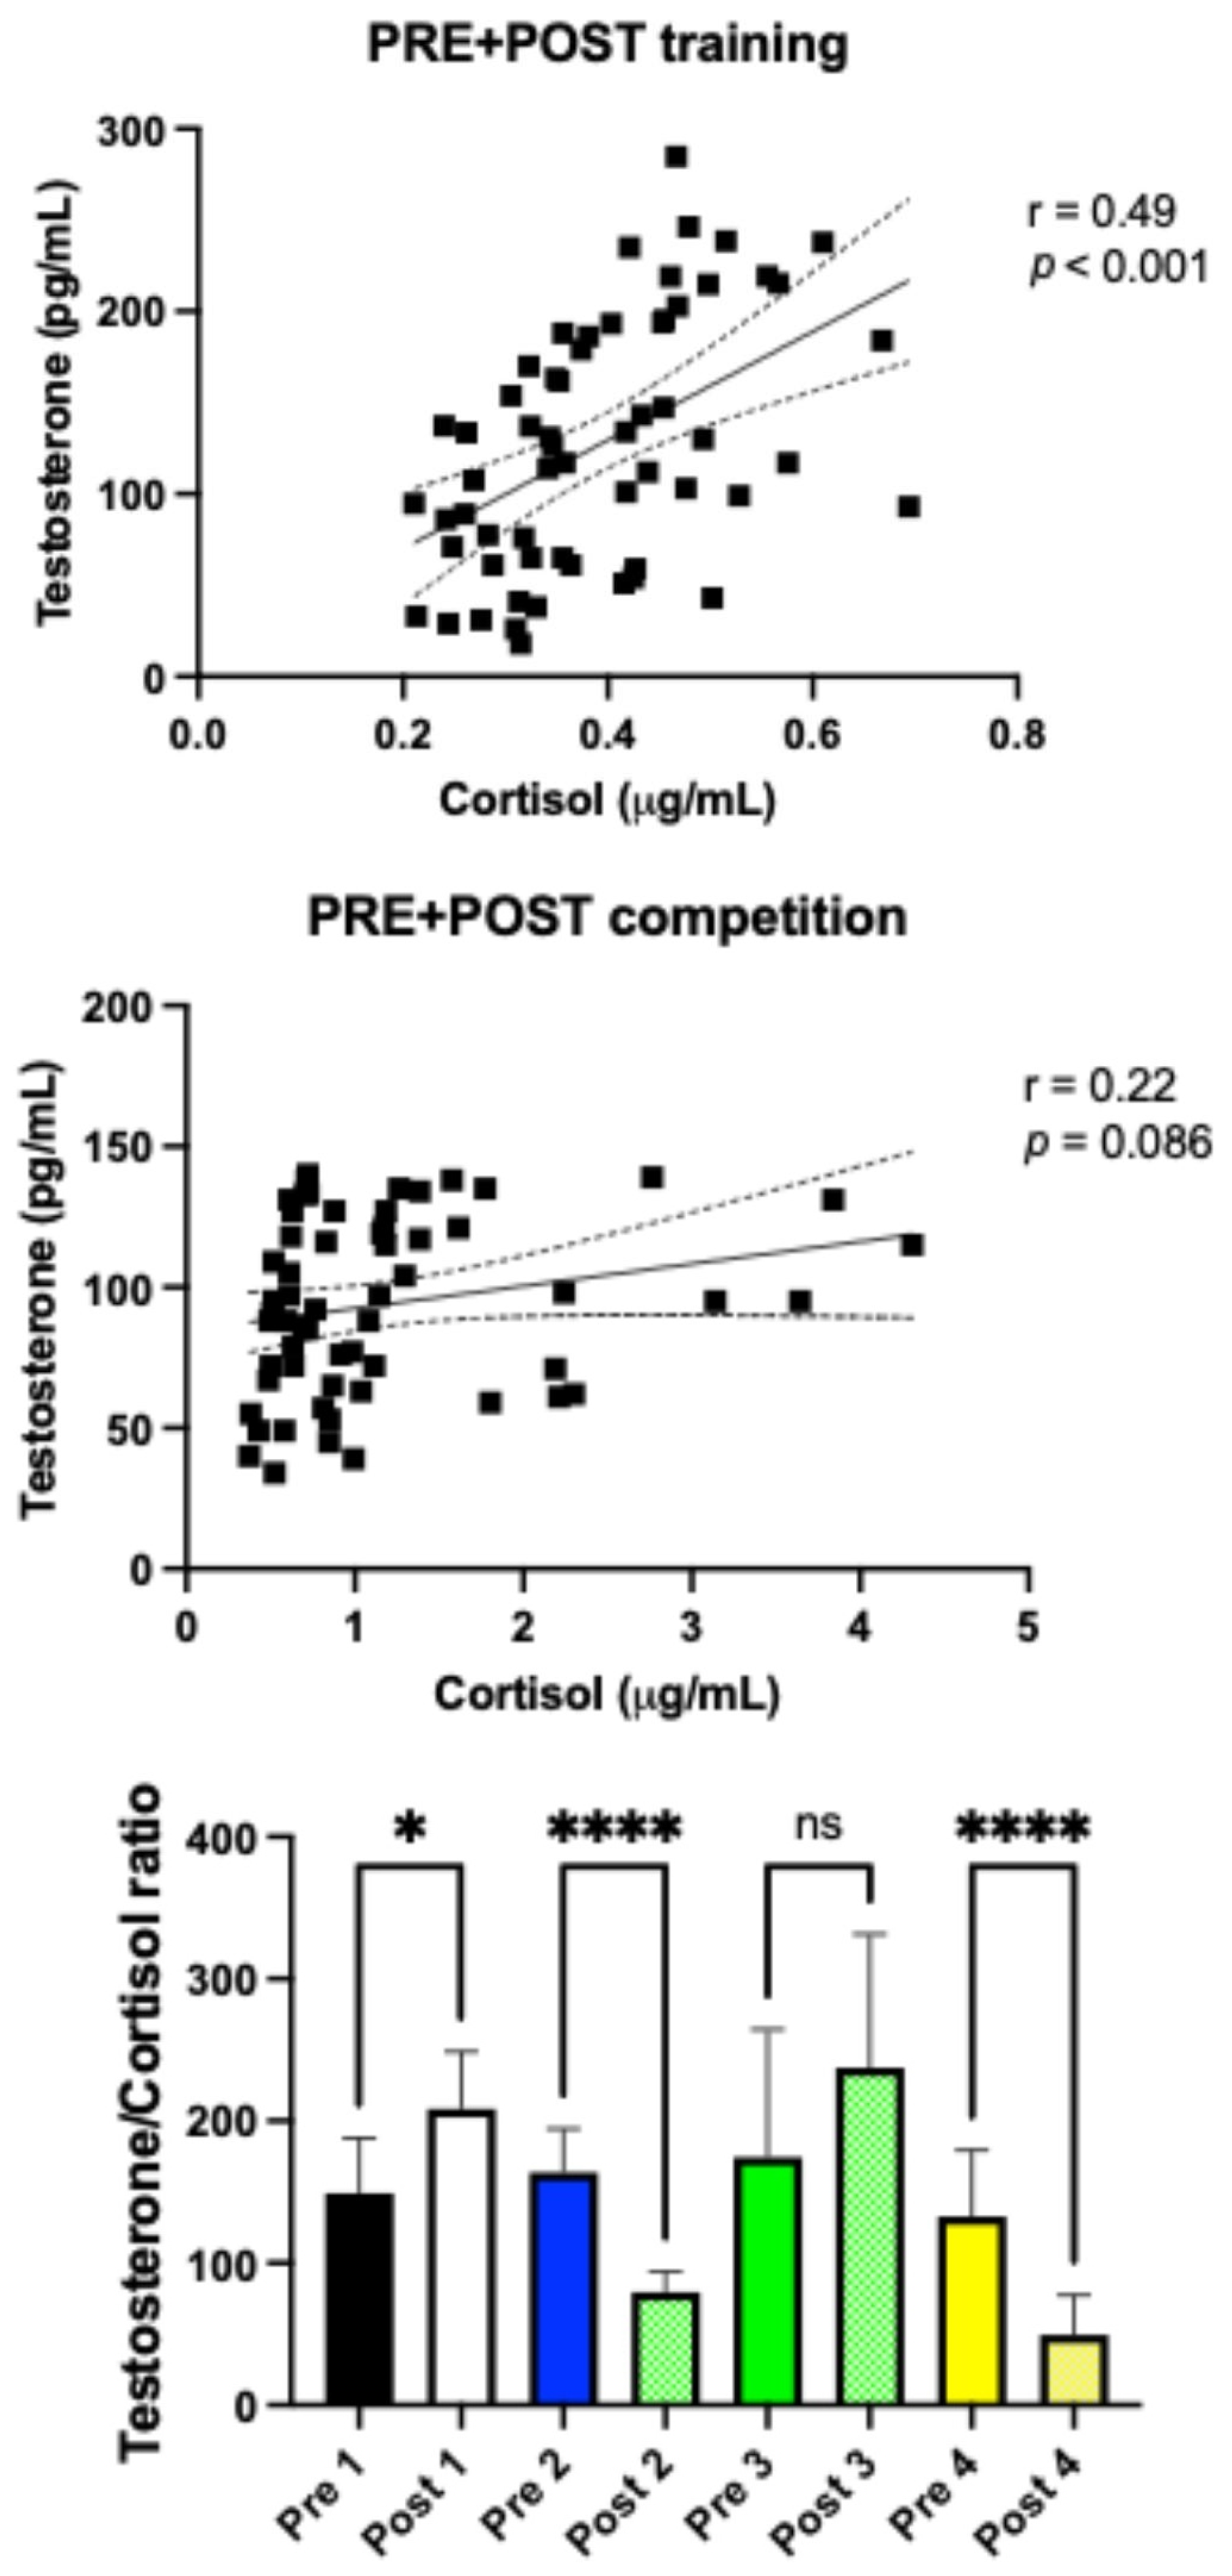
Within-session relationships between salivary testosterone and cortisol, together with the testosterone-to-cortisol (T/C) ratio, are presented in Figure 4. During training, a significant moderate positive correlation between testosterone and cortisol was observed from PRE to POST (r = 0.49, p < 0.001), indicating coordinated regulation of anabolic and catabolic hormonal responses under conditions of lower psychosocial stress.
In contrast, during competition, the association between testosterone and cortisol was weaker and did not reach statistical significance (r = 0.22, p = 0.086), with greater dispersion of individual data points. This pattern suggests a reduced coupling between these hormonal axes under competitive conditions, despite the higher overall cortisol levels observed.
Analysis of the T/C ratio further supported these findings. Training sessions were characterized by relatively higher and more stable T/C values, whereas competition showed a reduction in the ratio and increased inter-individual variability. This shift reflects a relative predominance of catabolic activity during competition, driven primarily by elevated cortisol in the absence of a corresponding increase in testosterone.
Collectively, these results indicate that competition not only amplifies endocrine responses but also alters the functional relationship between testosterone and cortisol, contributing to a distinct hormonal profile compared with training.

3.4. Cortisol-IgA and Testosterone-IgA Coupling Within Sessions

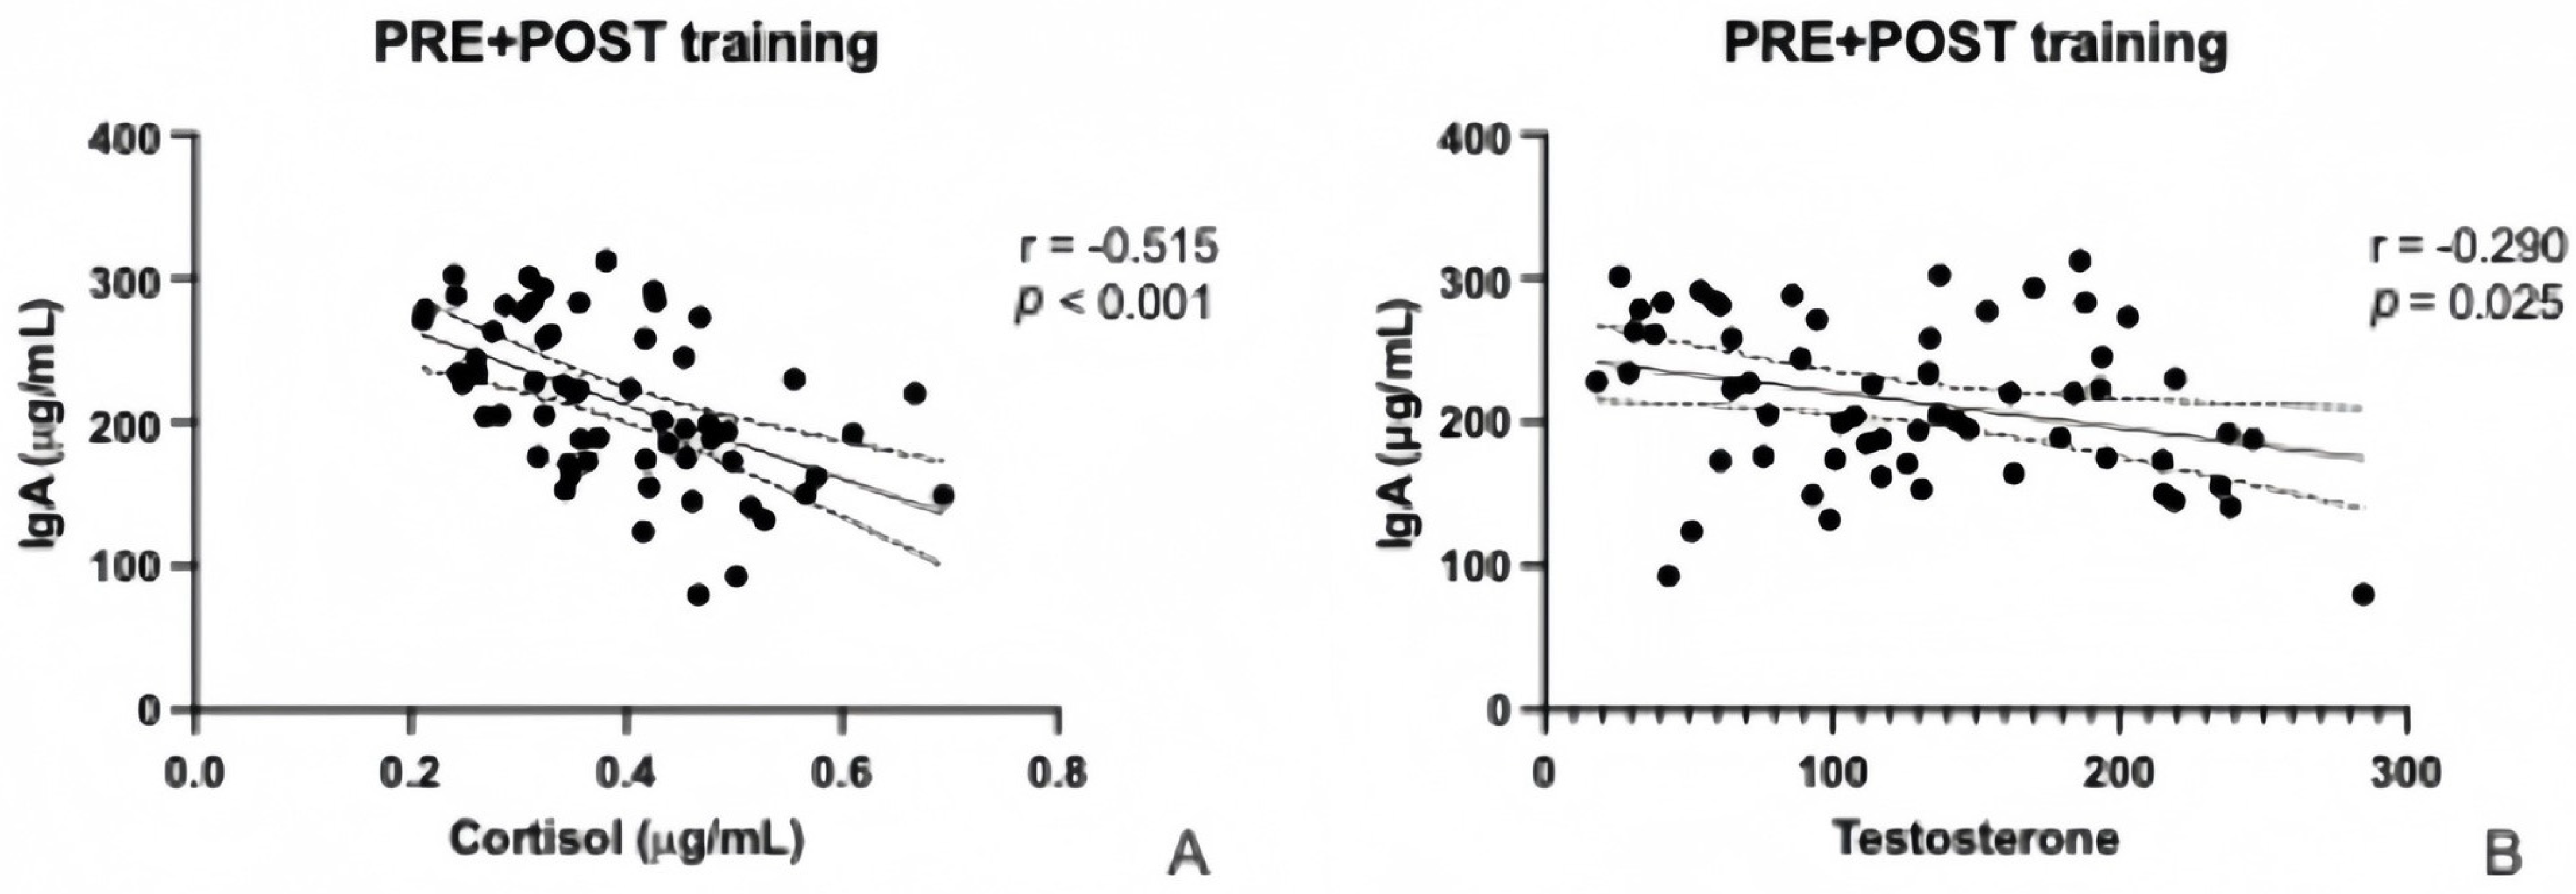
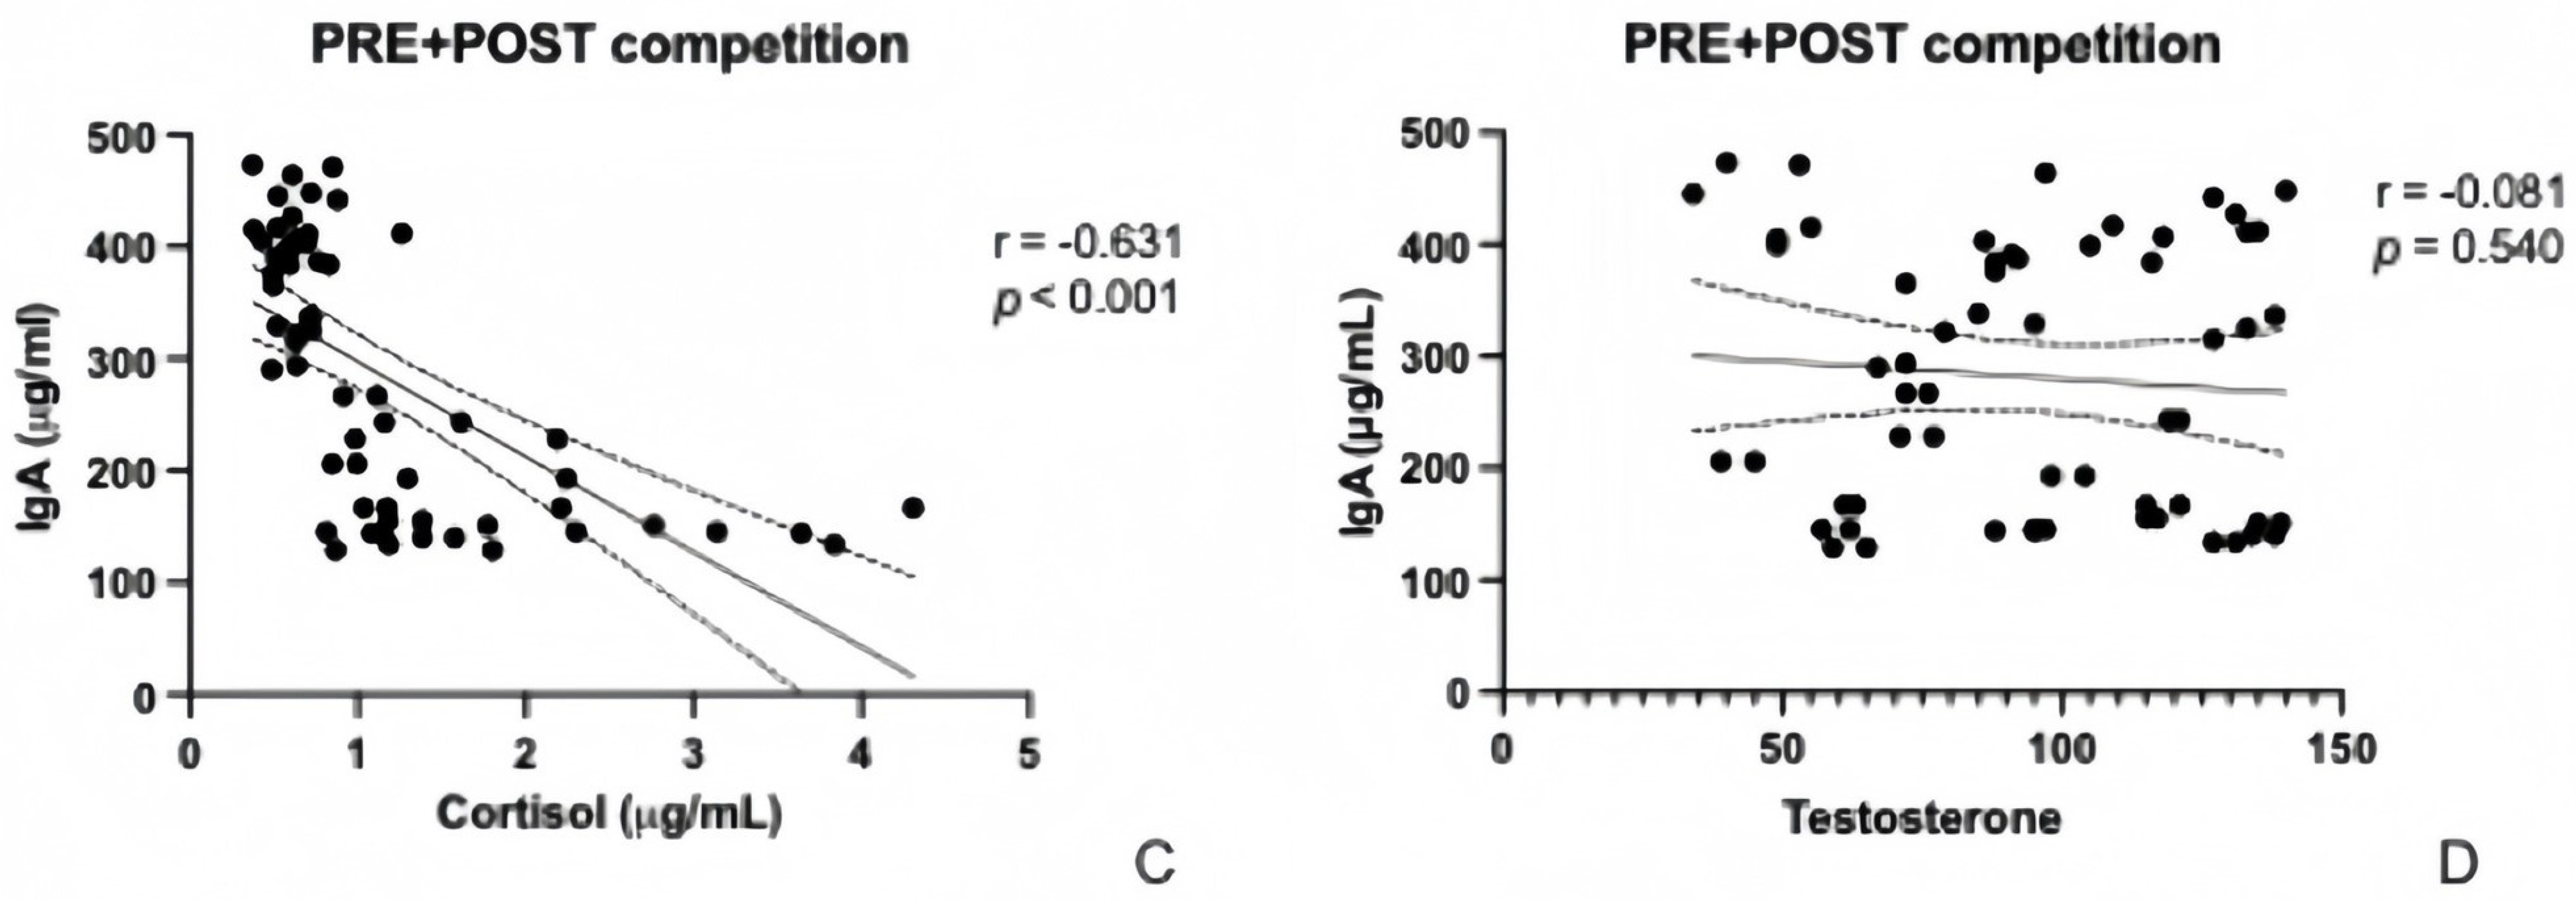
Within-session associations between salivary cortisol, testosterone, and IgA are presented in Figure 5. During training, a significant moderate inverse correlation was observed between cortisol and IgA from PRE to POST (r = −0.515, p < 0.001), indicating that increases in HPA axis activity were associated with reductions in mucosal immune markers. This relationship was even stronger during competition (r = −0.631, p < 0.001), suggesting a more pronounced coupling between cortisol elevation and IgA suppression under worsened psychosocial stress.
In contrast, testosterone–IgA associations differed markedly between conditions. During training, a significant but weaker inverse correlation was observed (r = −0.290, p = 0.025), indicating a modest relationship between anabolic signaling and mucosal immunity. However, during competition, this association was abolished (r = −0.081, p = 0.540), reflecting a lack of coupling between testosterone and IgA responses under competitive conditions.
Collectively, these findings indicate that cortisol–IgA relationships remain robust and are amplified during competition, whereas testosterone–IgA coupling is weakened or lost. This differential pattern suggests that competition selectively strengthens catabolic–immune interactions while disrupting anabolic–immune coordination, contributing to a context-dependent reorganization of neuroendocrine–immune integration.

3.5. Cytokine–Cortisol Coupling Within Sessions

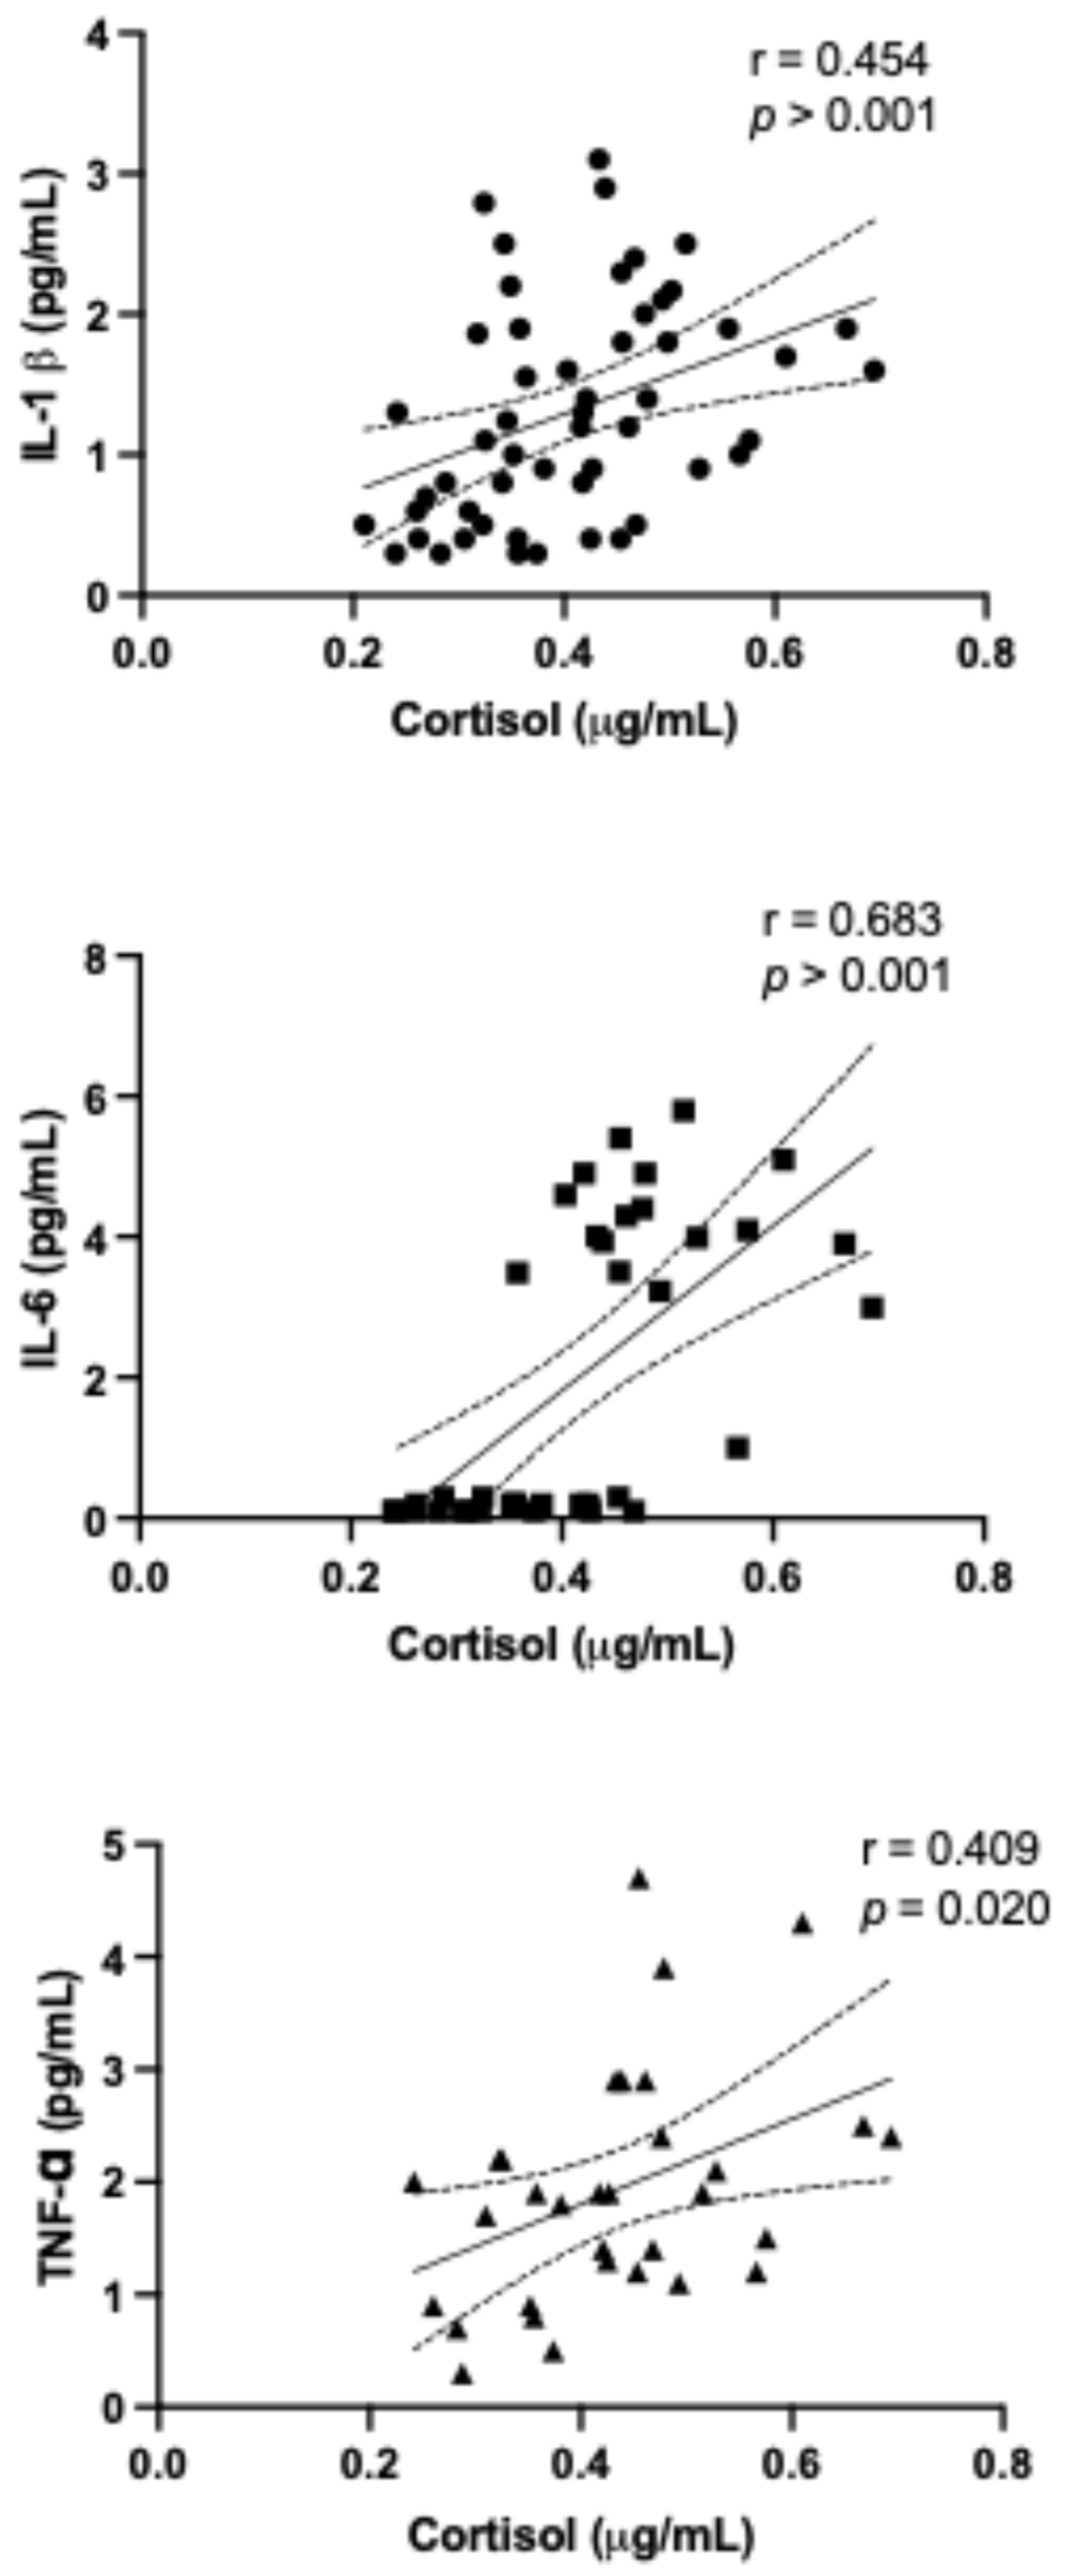
To further explore neuroendocrine–immune integration, within-session associations between salivary cortisol and cytokine concentrations were examined. During training, several cytokines demonstrated positive correlations with cortisol at both PRE and POST time points (Figure 6). These associations suggest coordinated activation of endocrine and immune signaling pathways under conditions of lower psychosocial load.
In contrast, correlation patterns during competition were more heterogeneous. While competition elicited larger absolute cytokine and cortisol responses, the strength and consistency of within-session associations were attenuated for some markers, suggesting partial decoupling under high psychosocial load. This pattern may reflect differential timing, saturation effects, or regulatory feedback mechanisms introduced by heightened anticipatory stress.

4. Discussion

The present study demonstrates that official competition elicits markedly stronger salivary cytokine and cortisol responses than matched training sessions in elite water polo players, accompanied by greater post-session IgA suppression. Together, these responses delineate an integrated psychophysiological stress signature that distinguishes competitive match play from ecologically similar training, despite broadly comparable physical demands. Under conditions of lower psychosocial load, the observed associations may reflect a coordinated activation of endocrine and immune signaling pathways [23]. In contrast, correlation patterns during competition appeared more heterogeneous. Although competition elicited larger absolute cytokine and cortisol responses, the strength and consistency of within-session associations were attenuated for some markers. This finding may indicate a partial decoupling of these systems under high psychosocial load. Such a pattern could be explained by differences in response kinetics, saturation effects, or regulatory feedback mechanisms associated with increased anticipatory stress.

4.1. Competition as an Amplifier of Neuroendocrine–Immune Activation

The consistently higher anticipatory and post-session cortisol concentrations observed during competition confirm that official matches impose a substantially greater HPA axis load than training. This finding aligns with extensive evidence showing that psychosocial stressors—such as outcome uncertainty, social evaluation, and performance accountability—potentiate cortisol release beyond that attributable to physical exertion alone [3,4,5]. Similar anticipatory cortisol elevations have been reported in elite athletes across individual and team sports, including swimming, rugby, and soccer, particularly in contexts where competitive salience is high [1,2,6].
The cytokine responses observed in the present study parallel this endocrine amplification. Although both training and competition induced post-session increases in salivary cytokines, competition was associated with substantially greater induction across the panel, including canonical pro-inflammatory mediators such as IL-6, TNF-α, and IL-1β. IL-6, in particular, exhibited pronounced sensitivity to competitive stress, consistent with its dual role as both a myokine released in response to muscular work and a stress-responsive cytokine influenced by neuroendocrine signaling [7,8,9,13]. The exaggerated IL-6 response during competition likely reflects the combined effects of high-intensity intermittent effort, physical contact, and heightened central stress drive.
These findings demonstrate that competition induces larger changes in cortisol and IgA compared with training and collectively support the concept that competition represents a qualitatively distinct physiological stimulus rather than a mere intensification of training load. Similar dissociations between training and competition have been reported in other high-contact and intermittent sports, where immune and endocrine perturbations are disproportionately amplified in competitive contexts [1,2,10,11,12].
These observations are consistent with findings in endurance sports such as cycling [25], where prolonged competitive load induces significant alterations in cortisol and testosterone dynamics and reflects sustained stress on both the HPA and HPG axes. Similarly, high-intensity efforts in rowing competitions have been shown to elicit marked increases in cortisol and acute immune redistribution, supporting the notion that competition represents a potent physiological stressor across endurance disciplines [25,26].

4.2. Mucosal Immunity, Oxidative Stress, and Illness Risk

The greater post-session suppression of salivary IgA during competition is of particular relevance from a health perspective. Salivary IgA is a key component of mucosal immune defense, and transient reductions following intense exercise have been linked to increased susceptibility to upper respiratory tract infections in athletes [10,13,14,15]. The magnified IgA decrease observed during competition suggests that repeated exposure to competitive stress, especially in congested match calendars, may meaningfully increase illness risk in water polo players.
Comparable trends have been reported in athletics-based studies, where competitive phases are associated with reductions in IgA and alterations in cortisol levels, suggesting increased susceptibility to transient immune perturbations under intensified load [27,28]. In contrast, findings in swimming appear more heterogeneous, with some studies reporting stable or even attenuated cortisol responses depending on exercise intensity and context, highlighting the variability of endocrine–immune interactions across disciplines [27,28].

4.3. Testosterone Dynamics and Anabolic–Catabolic Balance Under Competitive Stress

An additional relevant finding of the present study concerns the modulation of testosterone dynamics and its interaction with both cortisol and mucosal immunity. During training, a moderate positive association between testosterone and cortisol was observed, indicating coordinated activation of anabolic and catabolic endocrine pathways under conditions of substantial physical load but relatively lower psychosocial stress [29,30,31,32,33]. This pattern is consistent with integrated stress physiology models, in which multiple hormonal systems are co-activated to support energy mobilization, tissue turnover, and recovery.
In contrast, this association was attenuated during competition indicating a reduction in the strength and consistency of testosterone–cortisol coupling under heightened psychosocial load [34,35]. Notably, this occurred despite the marked increase in cortisol observed during competitive matches, suggesting that anabolic signaling does not scale proportionally with catabolic activation. Such divergence may reflect stress-related modulation of the hypothalamic–pituitary–gonadal axis [34,36,37], or a shift toward prioritization of immediate energy availability over anabolic maintenance in high-pressure contexts [34,36,37].
Further insight is provided by the analysis of testosterone–IgA relationships. During training, a weak but significant inverse association was observed, indicating a modest interaction between anabolic signaling and mucosal immune function [38,39]. In contrast, this relationship was not evident during competition, suggesting a loss of coordinated regulation between testosterone and immune markers under competitive stress. Importantly, cortisol–IgA coupling remained robust and was amplified during competition, highlighting the dominant role of HPA axis activation in mediating mucosal immune suppression [27,40].
Consistently, the testosterone-to-cortisol (T/C) ratio was reduced and more variable during competition, reflecting a shift toward catabolic predominance [27,40]. Together with the attenuation of testosterone–cortisol and testosterone–IgA associations, these findings suggest a context-dependent reorganization of endocrine–immune interactions. Specifically, competitive stress appears to preserve or strengthen catabolic–immune coupling while weakening anabolic integration, consistent with a partial decoupling of stress-regulatory systems under high psychosocial load [37].

4.4. Cytokine–Cortisol Coupling and Stress Integration

An important novel observation of this study is the presence of positive within-session correlations between cortisol and selected cytokines during training. This pattern suggests tightly coordinated regulation between HPA axis activation and immune signaling under conditions of substantial physical exertion but relatively moderate psychosocial stress. Such coupling is consistent with models of integrated stress physiology, in which glucocorticoids and cytokines act in concert to mobilize energy substrates, regulate inflammation, and facilitate recovery [7,8,17,18,19].
Interestingly, these associations appeared less consistent during competition, despite larger absolute responses. This apparent partial decoupling under high psychosocial load may reflect nonlinear dynamics, timing mismatches between endocrine and immune signaling, or saturation effects at higher stress levels. Similar phenomena have been described in both athletic and clinical settings, where excessive or repeated stress exposure disrupts otherwise coordinated neuroendocrine–immune crosstalk [20,21,22,23]. These findings warrant further investigation using higher-resolution sampling and modeling approaches.

4.5. Applied Implications for Monitoring and Load Management

From an applied standpoint, the integration of salivary cortisol, cytokines, and IgA represents a practical, non-invasive framework for monitoring athlete stress and recovery in elite water polo. Saliva-based biomarkers are particularly well suited to aquatic environments, where venous sampling is impractical and compliance with frequent testing is limited.
Multimarker profiling may allow practitioners to identify athletes experiencing disproportionate competitive stress responses, inform individualized load management strategies, and potentially mitigate illness risk associated with repeated mucosal immune suppression. Similar approaches have proven valuable in other elite sport settings, where biomarker-informed decision-making has been used to optimize performance while safeguarding athlete health [1,2,21,22].

4.6. Limitations and Strengths

Some limitations should be acknowledged. First, the study group is limited due to small sample size, lack of female participants and single team cohort, which may restrict the generalizability of the findings. These factors should be considered when interpreting the results, as neuroendocrine and immune responses may vary across different populations. Future studies including more diverse cohorts are warranted. Second, positional role, actual playing time, and fine-grained external load metrics were not explicitly modeled and should be incorporated into future mixed-effects or multilevel frameworks.
Nevertheless, the study has notable strengths, including high ecological validity, synchronized evening sampling to control for circadian effects, and a comprehensive multimarker approach spanning endocrine, and immune pathways. Importantly, the within-subject comparison of training and competition provides a powerful design for isolating the effects of competitive context.
Although blood sampling is generally considered the reference method for assessing endocrine and immune biomarkers, salivary sampling provides a noninvasive, stress-free, and field-applicable alternative that is particularly suitable in athletic settings. Importantly, salivary cortisol reflects the biologically active free fraction, and salivary cytokines and IgA have been widely used as indicators of mucosal immunity [24,39,41,42,43]. Nevertheless, differences in concentrations and kinetics between saliva and blood should be acknowledged [43], and future studies combining both matrices would provide a more comprehensive evaluation of neuroendocrine–immune interactions.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/biochem6030016/s1. Table S1. Health Screening Questionnaire.

Author Contributions

Conceptualization, N.N.T., A.S., D.M. and D.S.; methodology, N.N.T., M.C., D.M., L.N. and D.S.; validation, N.N.T., G.C., A.S., S.N., D.M., L.N. and D.S.; formal analysis, N.N.T., M.C., D.M., and D.S.; resources, M.C., L.N., and D.S.; data curation, N.N.T., A.S., and D.S.; writing—original draft preparation, D.S.; writing—review and editing, N.N.T., G.C., L.N. and D.S.; visualization, N.N.T., A.S., S.N., G.C., L.N. and D.S.; supervision, L.N. and D.S. All authors have read and agreed to the published version of the manuscript.

Funding

This research did not receive any specific grant from funding agencies in the public, commercial, or not-for-profit sectors.

Institutional Review Board Statement

The study was approved by the Ethical Committee of the University of Genoa (CERA 2024/34, 25 March 2024), and all participants provided written informed consent. The study was conducted following the Declaration of Helsinki II.

Informed Consent Statement

Informed consent was obtained from all subjects involved in the study. The authors assert that all procedures contributing to this work comply with the ethical standards of the relevant national and institutional committees on human experimentation and with the Helsinki Declaration of 1975, as revised in 2000.

Data Availability Statement

Data will be made available on reasonable request.

Acknowledgments

The authors would like to sincerely thank the water polo players who voluntarily participated in this study for their commitment, collaboration, and willingness to take part in repeated physiological and psychological assessments.

Conflicts of Interest

The authors declare no conflicts of interest. The authors alone are responsible for the content and writing of this manuscript, and no personal, financial, or professional relationships influenced the design, conduct, analysis, or reporting of this study.

References

  1. Twist, C.; Highton, J.; Daniels, M.; Mill, N.; Close, G. Player Responses to Match and Training Demands During an Intensified Fixture Schedule in Professional Rugby League: A Case Study. Int. J. Sports Physiol. Perform. 2017, 12, 1093–1099. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Thorpe, R.T.; Strudwick, A.J.; Buchheit, M.; Atkinson, G.; Drust, B.; Gregson, W. Monitoring Fatigue during the In-Season Competitive Phase in Elite Soccer Players. Int. J. Sports Physiol. Perform. 2015, 10, 958–964. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Dickerson, S.S.; Kemeny, M.E. Acute Stressors and Cortisol Responses: A Theoretical Integration and Synthesis of Laboratory Research. Psychol. Bull. 2004, 130, 355–391. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Salvador, A.; Costa, R. Coping with Competition: Neuroendocrine Responses and Cognitive Variables. Neurosci. Biobehav. Rev. 2009, 33, 160–170. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Hellhammer, D.H.; Wüst, S.; Kudielka, B.M. Salivary Cortisol as a Biomarker in Stress Research. Psychoneuroendocrinology 2009, 34, 163–171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Crewther, B.T.; Cook, C.; Cardinale, M.; Weatherby, R.P.; Lowe, T. Two Emerging Concepts for Elite Athletes—The Short-Term Effects of Testosterone and Cortisol on the Neuromuscular System and the Dose-Response Training Role of these Endogenous Hormones. Sports Med. 2011, 41, 103–123. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Sternberg, E.M. Neural Regulation of Innate Immunity: A Coordinated Nonspecific Host Response to Pathogens. Nat. Rev. Immunol. 2006, 6, 318–328. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Dhabhar, F.S. Effects of Stress on Immune Function: The Good, the Bad, and the Beautiful. Immunol. Rev. 2014, 58, 193–219. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Gleeson, M. Immune Function in Sport and Exercise. J. Appl. Physiol. 2007, 103, 693–699. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Neville, V.; Gleeson, M.; Folland, J.P. Salivary IgA as a Risk Factor for Upper Respiratory Infections in Elite Professional Athletes. Med. Sci. Sports Exerc. 2008, 40, 1228–1236. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Filaire, E.; Alix, D.; Ferrand, C.; Verger, M. Psychophysiological stress in tennis players during the first single match of a tournament. Psychoneuroendocrinology 2009, 34, 150–157. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Peake, J.M.; Neubauer, O.; Della Gatta, P.A.; Nosaka, K. Muscle Damage and Inflammation during Recovery from Exercise. J. Appl. Physiol. 2017, 122, 559–570. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Fischer, C.P. Interleukin-6 in acute exercise and training: What is the biological relevance? Exerc. Immunol. Rev. 2006, 12, 6–33. [Google Scholar] [PubMed]
  14. Zhang, Q.; Dai, J.; Ali, A.; Chen, L.; Huang, X. Roles of Bioavailable Iron and Calcium in Coal Dust-induced Oxidative Stress: Possible Implications in Coal Workers’ Lung Disease. Free Radic. Res. 2002, 36, 285–294. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Powers, S.K.; Jackson, M.J. Exercise-Induced Oxidative Stress: Cellular Mechanisms and Impact on Muscle Force Production. Physiol. Rev. 2008, 88, 1243–1276. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. Yoneda, M.; Saitoh, K. Nonspecific Effects of Gap Paradigm on Swallowing. Physiol. Behav. 2017, 169, 141–146. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Rohleder, N. Stimulation of Systemic Low-Grade Inflammation by Psychosocial Stress. Psychosom. Med. 2014, 76, 181–189. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Slavich, G.M.; Irwin, M.R. From Stress to Inflammation and Major Depressive Disorder: A Social Signal Transduction Theory of Depression. Psychol. Bull. 2014, 140, 774–815. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Joseph, P.V.; Davidson, H.R.; Boulineaux, C.M.; Fourie, N.H.; Franks, A.T.; Abey, S.K.; Henderson, W.A. Eating Behavior, Stress, and Adiposity: Discordance Between Perception and Physiology. Biol. Res. Nurs. 2018, 20, 531–540. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Weiss, M.; Newman, A.; Whitmore, C.; Weiss, S. One Hundred and Fifty Years of Sprint and Distance Running—Past Trends and Future Prospects. Eur. J. Sport Sci. 2016, 16, 393–401. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Hecksteden, A.; Kraushaar, J.; Scharhag-Rosenberger, F.; Theisen, D.; Senn, S.; Meyer, T. Individual Response to Exercise Training—A Statistical Perspective. J. Appl. Physiol. 2015, 118, 1450–1459. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Kellmann, M.; Bertollo, M.; Bosquet, L.; Brink, M.; Coutts, A.J.; Duffield, R.; Erlacher, D.; Halson, S.L.; Hecksteden, A.; Heidari, J.; et al. Recovery and Performance in Sport: Consensus Statement. Int. J. Sports Physiol. Perform. 2018, 13, 240–245. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Nogueira, J.M.; Simães, C.; Morais, C.; Mansell, P.; Gomes, A.R. Coping Strategies Before Competition: The Role of Stress, Cognitive Appraisal, and Emotions. Sports 2025, 13, 366. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Nikousokhan Tayyar, N.; Naim, S.; Strangio, A.; Mugia, D.; Nanni, L.; Saverino, D. Competitive Stress Elicits Distinct Psychophysiological and Immunological Responses in Elite Water Polo Players. Preprints 2026, 2026050418. [Google Scholar] [CrossRef] [Scilit]
  25. Simonetto, L.; Fiorella, P.; Impellizzeri, F.M.; Giorgi, A.; Bonifazi, M. Testosterone and cortisol in 93 elite road cyclists during a 10-day stage race: Relationship with final ranking. Sport Sci. Health 2016, 12, 407–413. [Google Scholar] [CrossRef] [Scilit]
  26. Ha, S.-M.; Ha, M.-S.; Lee, M. Acute endocrine, immune, and muscle damage responses following a 2000-m rowing time trial in elite male athletes. Front. Physiol. 2025, 16, 1712471. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Hejazi, K.; Hosseini, S.R. Influence of selected exercise on serum immunoglobulin, testosterone and cortisol in semi-endurance elite runners. Asian J. Sports Med. 2012, 3, 185–192. [Google Scholar] [PubMed] [PubMed Central]
  28. Cichoń-Woźniak, J.; Dziewiecka, H.; Ostapiuk-Karolczuk, J.; Mydłowska, M.; Szymańczuk, M.; Skarpańska-Stejnborn, A. Exercise-induced oxidative and hematological responses in adolescent female swimmers during the luteal phase. Front. Physiol. 2026, 17, 1705876. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Minuzzi, L.G.; Rama, L.; Chupel, M.U.; Rosado, F.; Kuga, G.K.; Gaspar, R.C.; Muñoz, V.R.; Pauli, J.R.; Paiva, A.; Teixeira, A.M. Immune-endocrine responses and physical performance of master athletes during the sports season. J. Cell Biochem. 2019, 120, 5551–5557. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Crewther, B.T.; Serpell, B.; Potts, N.; Kilduff, L.; Cook, C.J. Dose-response and time-lagged effect of daily training load on athlete well-being during an international rugby series. Biol. Sport 2025, 42, 39–45. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Mbiydzenyuy, N.E.; Qulu, L.A. Stress, hypothalamic-pituitary-adrenal axis, hypothalamic-pituitary-gonadal axis, and aggression. Metab. Brain Dis. 2024, 39, 1613–1636. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Zueger, R.; Annen, H.; Ehlert, U. Testosterone and cortisol responses to acute and prolonged stress during officer training school. Stress 2023, 26, 2199886. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Friedl, K.E.; Nindl, B.C.; Potter, A.W. Stress-associated testosterone suppression: Central adaptation or hypogonadism? J. Clin. Endocrinol. Metab. 2026, dgag181. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Domes, G.; Linnig, K.; von Dawans, B. Gonads under stress: A systematic review and meta-analysis on the effects of acute psychosocial stress on gonadal steroids secretion in humans. Psychoneuroendocrinology 2024, 164, 107004. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Son, Y.L.; Ubuka, T.; Tsutsui, K. Regulation of stress response on the hypothalamic-pituitary-gonadal axis via gonadotropin-inhibitory hormone. Front. Neuroendocrinol. 2022, 64, 100953. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Demori, I.; Siriya, S.; Burlando, B. Loop Modeling of the Reciprocal Inhibition Between HPA and HPG Endocrine Axes Reveals Transitions to Bistability and Critical Bifurcation Parameters. Appl. Sci. 2025, 15, 10483. [Google Scholar] [CrossRef] [Scilit]
  37. Trumble, B.C.; Blackwell, A.D.; Stieglitz, J.; Thompson, M.E.; Maldonado Suarez, I.; Kaplan, H.; Gurven, M. Associations between male testosterone and immune function in a pathogenically stressed forager-horticultural population. Am. J. Phys. Anthropol. 2016, 161, 494–505. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Morgans, R.; Oliveira, R.; Rhodes, D.; Orme, P.; Ceylan, H.I.; González-Fernández, F.T.; Linán-González, A.; Moreira, A. Does elite European match-play affect salivary immunoglobulin-A and cortisol in soccer players? The influence of playing status and match outcome. Front. Physiol. 2024, 15, 1253417. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Neves, R.S.; da Silva, M.A.R.; de Rezende, M.A.C.; Caldo-Silva, A.; Pinheiro, J.; Santos, A.M.C. Salivary Markers Responses in the Post-Exercise and Recovery Period: A Systematic Review. Sports 2023, 11, 137. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. De Luccia, T.P.B. Use of the Testosterone/Cortisol Ratio Variable in Sports. Open Sports Sci. J. 2016, 9, 104–113. [Google Scholar] [CrossRef] [Scilit]
  41. Francavilla, V.C.; Vitale, F.; Ciaccio, M.; Bongiovanni, T.; Marotta, C.; Caldarella, R.; Todaro, L.; Zarcone, M.; Muratore, R.; Bellia, C.; et al. Use of Saliva in Alternative to Serum Sampling to Monitor Biomarkers Modifications in Professional Soccer Players. Front. Physiol. 2018, 9, 1828. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Jankowski, J.; Nijakowski, K. Salivary Immunoglobulin a Alterations in Health and Disease: A Bibliometric Analysis of Diagnostic Trends from 2009 to 2024. Antibodies 2024, 13, 98. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Constantin, V.; Luchian, I.; Goriuc, A.; Budala, D.G.; Bida, F.C.; Cojocaru, C.; Butnaru, O.-M.; Virvescu, D.I. Salivary Biomarkers Identification: Advances in Standard and Emerging Technologies. Oral 2025, 5, 26. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Study design and sampling timeline. Schematic representation of the within-subject experimental design. Each participant completed one standardized training session (TRAIN) and one official competitive match (COMP), both conducted in the evening. Saliva samples were collected at PRE (15–20 min before session start) and POST (15–20 min after session completion).
Biochem 06 00016 g001
Figure 2. Cortisol and IgA responses to training and competition. Changes in salivary cortisol (upper), testosterone (middle) and IgA (lower) from PRE to POST during training (TRAIN) and competition (COMP). Data are presented as mean ± SEM. Competition elicited significantly higher anticipatory and post-session cortisol concentrations and a significantly greater post-session reduction in IgA compared with training. *** p = 0.001; **** p < 0.0001; ns: no significant.
Biochem 06 00016 g002aBiochem 06 00016 g002b
Figure 3. Salivary cytokine responses to training and competition. PRE–POST changes in salivary cytokine concentrations during training and competition. Data are shown as mean ± SEM. All cytokines increased post-session in both conditions, with significantly greater induction during competition, indicating amplified immune activation under competitive stress. * p = 0.0255; ** p = 0.099; *** p = 0.001; **** p < 0.0001.
Biochem 06 00016 g003
Figure 4. Testosterone–cortisol associations within sessions and testosterone ration. Scatterplots illustrating within-session associations between salivary testosterone and cortisol concentrations during training and competition from PRE to POST. A significant positive correlation was observed during training (r = 0.49, p < 0.001), whereas the association during competition was weaker and not statistically significant (r = 0.22, p = 0.086). Bar plots represent the testosterone-to-cortisol (T/C) ratio across conditions, showing higher and more stable values during training and reduced, more variable values during competition, consistent with a shift toward catabolic predominance. Data are presented as mean ± SEM; p < 0.05 was considered statistically significant. * p = 0.0126, **** p < 0.0001; ns: no significant. Solid lines indicate the best-fit line, dash lines indicate the 95% confidence results.
Biochem 06 00016 g004
Figure 5. Scatterplots illustrating PRE–POST within-session correlations between salivary cortisol and IgA, and testosterone and IgA, during training and competition sessions. Cortisol–IgA associations were significant and inverse in both training (r = −0.515, p < 0.001) and competition (r = −0.631, p < 0.001), with stronger coupling observed under competitive conditions (panel (A,B) respectively). Testosterone–IgA correlations were weaker and significant during training (r = −0.290, p = 0.025) but not during competition (r = −0.081, p = 0.540) (panel (C,D) respectively). These results indicate preserved and amplified HPA–immune coupling alongside disrupted anabolic–immune associations during competition. p < 0.05 was considered statistically significant. Solid lines indicate the best-fit line, dash lines indicate the 95% confidence results.
Biochem 06 00016 g005aBiochem 06 00016 g005b
Figure 6. Cytokine–cortisol associations within sessions. Scatterplots depicting within-session correlations between salivary cortisol and selected cytokines during training and competition. Spearman correlation coefficients (r) and 95% confidence intervals are shown. Positive associations were more consistent during training and attenuated during competition, suggesting altered neuroendocrine–immune coupling under high psychosocial load. p values lower than 0.05 were considered as significant. Solid lines indicate the best-fit line, dash lines indicate the 95% confidence results.
Biochem 06 00016 g006
Table 1. Cortisol, testosterone, and IgA across sessions.
Pre 1Post 1Pre 2Post 2Pre 3Post 3Pre 4Post 4
Cortisol (μg/mL)
Minimum0.21110.34340.37440.81310.21300.31800.51800.9160
Maximum0.46830.66790.72241.7720.42700.69401.2624.309
Range0.25720.32450.34800.95920.21400.37600.74403.393
Mean0.33590.48310.55751.1810.30480.44570.71652.285
Std. Deviation0.075990.090150.11500.27390.063050.10320.19141.072
Testosterone (pg/mL)
Minimum20.0045.0040.0045.0018.0043.0034.0039.00
Maximum95.00145.0140.0135.089.00143.0138.0139.0
Range75.00100.0100.090.0071.00100.0104.0100.0
Mean52.07101.993.8094.8751.07100.693.1394.20
Std. Deviation22.8429.3132.7230.2822.0830.8432.3631.70
IgA (μg/mL)
Minimum189.080.00223.093.00290.0129.0294.0107.0
Maximum312.0230.0301.0205.0473.0267.0471.0229.0
Range123.0150.078.00112.0183.0138.0177.0122.0
Mean252.8172.3262.9168.4398.7174.3379.6178.1
Std. Deviation38.5038.5626.1831.8148.3443.1554.1038.59
Table 2. Cytokine descriptive statistics.
Pre 1Post 1Pre 2Post 2Pre 3Post 3Pre 4Post 4
IL-1 β (pg/mL)
Minimum0.3001.0000.2001.5500.2000.9000.5002.000
Maximum1.0002.5001.0003.4001.3003.1001.7004.020
Range0.7001.5000.8001.8501.1002.2001.2002.020
Mean0.5401.8400.6402.3430.6401.8470.8402.910
Std. Deviation0.2380.4720.2200.52930.3160.6790.3000.641
IL-6 (pg/mL)
Minimum0.1001.0000.10003.0000.100013.200.200019.20
Maximum0.3005.8000.30004.4000.300026.200.600028.80
Range0.2004.8000.20001.4000.200013.000.40009.600
Mean0.1634.4130.17503.7690.200021.380.312524.44
Std. Deviation0.0741.5010.0890.4780.07564.2110.13564.042
TNF-α (pg/mL)
Minimum0.5001.2000.3001.1000.7001.5000.7002.100
Maximum2.2004.7002.2002.9001.6007.8002.0006.700
Range1.7003.5001.9001.8000.9006.3001.3004.600
Mean1.3252.8501.3882.1501.0755.2001.4383.800
Std. Deviation0.6101.3350.6730.6370.2822.2310.5211.595
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.