


Abstract
The three-tiered microbial food chain without maintenance under leachate recirculation is the subject of a mathematical seven-dimensional dynamical system that is proposed in this work. This model captures the complex interactions between chlorophenol degraders, phenol degraders, and methanogens in the presence of hydrogen inhibition. The implementation allows for investigation of how hydrogen levels affect the overall system dynamics and phenol production. There is a thorough qualitative analysis provided. A stability analysis of equilibrium points is performed. It is demonstrated that the persistence of the three bacteria is correlated with the existence of the positive equilibrium point, assuming some monotonicity properties on the growth rates. Asymptotic coexistence is satisfied, although periodic orbit possibilities are not ruled out. In order to decrease the amount of organic materials within the reactor, we suggest an optimal strategy on the rate of leachate recirculation in the second stage. Lastly, we offer a few numerical investigations that support and strengthen the theoretical conclusions.
MSC:
34K20; 34D23; 37B25; 37N25; 49J15; 92D25; 93A30
1. Introduction
A set of biological activities known as anaerobic digestion occurs when bacteria break down biodegradable materials without the presence of oxygen. Biogas, liquid digestate, and solid digestate are the end products of this process. Swamp gas is created by a similar natural process that takes place in wetlands and marshes. Landfill gas is also produced by the mostly anaerobic breakdown of the organic fraction in landfills. Methane, carbon dioxide, and hydrogen sulfide are present in landfill gas, biogas, and swamp gas, though in different proportions. There are four steps in this biological process: hydrolysis, acetogenesis, acidogenesis, and methanogenesis. The initial stage of turning organic material into biogas is hydrolysis. In order for the following group of bacteria to continue processing the material, some bacteria in this stage convert organic polymers, such as polysaccharides, into simple sugars. The second stage of turning organic material into biogas is called acidogenesis. Simple sugars and amino acids are transformed into carbon dioxide, hydrogen, ammonia, and organic acids at this step by specific bacteria known as acidogenic bacteria. The third stage in turning organic materials into biogas is called acetogenesis. At this point, the organic acids are changed into acetic acid, carbon dioxide, and hydrogen by specific bacteria known as acetogenic bacteria. The last stage of turning organic resources into biogas is called methanogenesis. The intermediate products created in the previous stages are transformed into biogas (mostly carbon dioxide and methane) in this stage by specific single-celled organisms known as methanogens. Digestate, the solid and liquid residue left over from this process, includes dead bacteria and materials that the microorganisms cannot consume. Anaerobic digestion can use a variety of feedstocks, including manure, industrial wastewater, municipal solid waste (MSW), municipal wastewater, fats, oils, and greases, food scraps, sludges, etc. Municipal solid waste (MSW) can be valorized through anaerobic digestion to produce digestate and biogas, which are organic soil amendments and renewable energy sources, respectively. When phenols, which are persistent pollutants found in MSW, are added to soil together with digestate, they can harm microbiota and prevent the anaerobic digestion process. Determining the anaerobic digestion operating parameters that permit the full breakdown of phenol is then crucial. Oil refineries, coking plants, chemical companies, and the production of polymeric resins all frequently release phenol as a pollutant. The US Environmental Protection Agency (EPA) designated phenol as a priority contaminant. Due to the presence of a big hydrocarbon group, phenol is somewhat soluble in water. We may therefore draw the conclusion that phenol is somewhat soluble in water and that this solubility results from an intermolecular hydrogen bond that forms between the water and the hydrogen atom in the hydroxyl group. Anaerobic wastewater treatment is hampered by phenol’s inhibitory effects. Several works studied the dynamic modeling of syntrophic interactions in anaerobic digestion [1,2,3,4]. Leachate is created when water seeps through solid waste, releasing soluble substances and waste breakdown products. Pollutants from solid waste are leached into the water when it flows through a landfill. Leaching of naturally soluble materials, leaching of soluble chemical products or biological reactions, fine washout, and colloids are some of the mechanisms used to remove contaminants [5]. In addition to substituted and chlorinated phenols, phenol and cresols are among the phenolic chemicals identified in the leachate [6]. Solvents and heat treatment have an impact on the antioxidant activity and soluble and insoluble phenolic components of immature calamondin [7]. The paper presents a comprehensive mathematical model to study the dynamics of a three-tiered microbial food web in a chemostat under leachate recirculation. The model captures interactions between chlorophenol degraders, phenol degraders, and methanogens, incorporating hydrogen inhibition effects. This work can make a valuable contribution to the mathematical modeling of microbial food webs in bioreactors. Its theoretical depth and innovative optimal control approach are valuable elements. Addressing the noted weaknesses, particularly by linking the model to experimental data and discussing practical implementation, would further enhance its impact. A seven-dimensional mathematical dynamical system for the three-tiered microbial food web under leachate recirculation is proposed in this research. The intricate relationships between methanogens, phenol degraders, and chlorophenol degraders in the presence of hydrogen inhibition are captured by this model.
This research paper is structured as follows: We introduce a seven-dimensional dynamical system that describes the three-tiered microbial food chain under the leachate recirculation in Section 2. The various hypotheses regarding the rates of bacterial growth, the proof of the solution’s positivity and boundedness and the definition of the steady states are all included in this section. Several preliminary results are introduced in Section 3. The seven-dimensional dynamical system is effectively reduced to a three-dimensional system in Section 4, simplifying analysis while retaining biological relevance. We discuss the existence and the local and global stability of the reduced dynamics’ equilibria in relation to the bacterial growth rates and the operating parameters (dilution rate and input concentrations). The persistence of the main seven dimensions dynamics is covered in Section 5. By reducing the amount of organic matter within the reactor and maintaining an optimal leachate recirculation rate, we suggest an optimal control technique in Section 6. For both the direct and optimum control problems, we present a number of numerical tests in Section 7 that confirm the key theoretical findings. In Section 8, we conclude the paper with a brief statement.
2. Mathematical Model
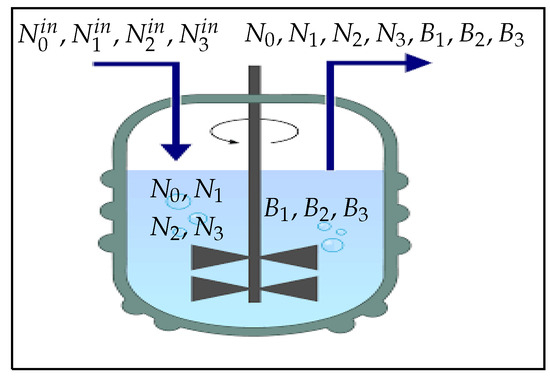
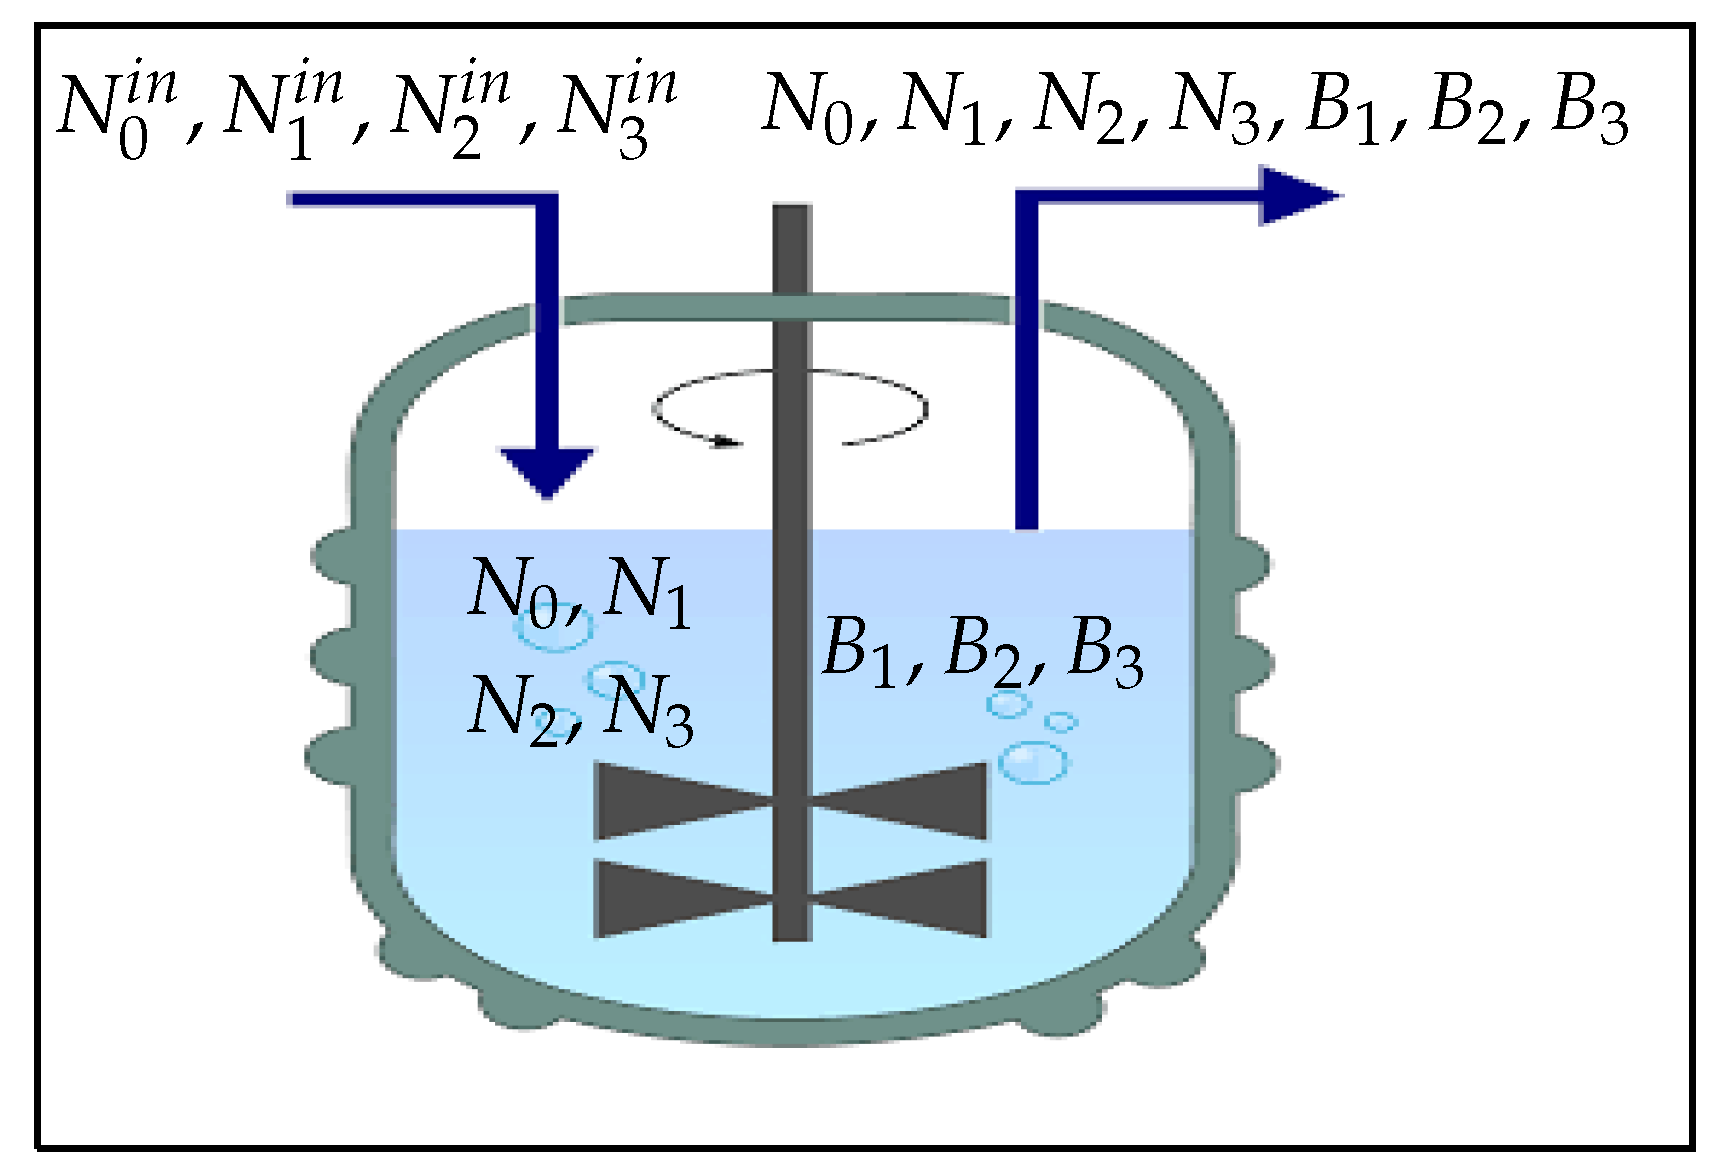
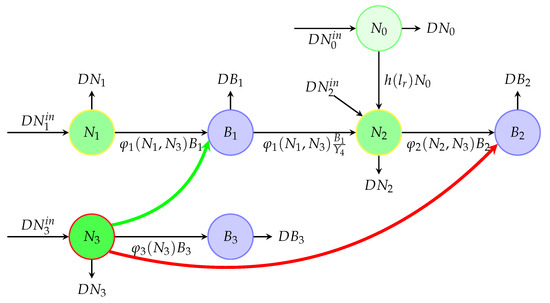
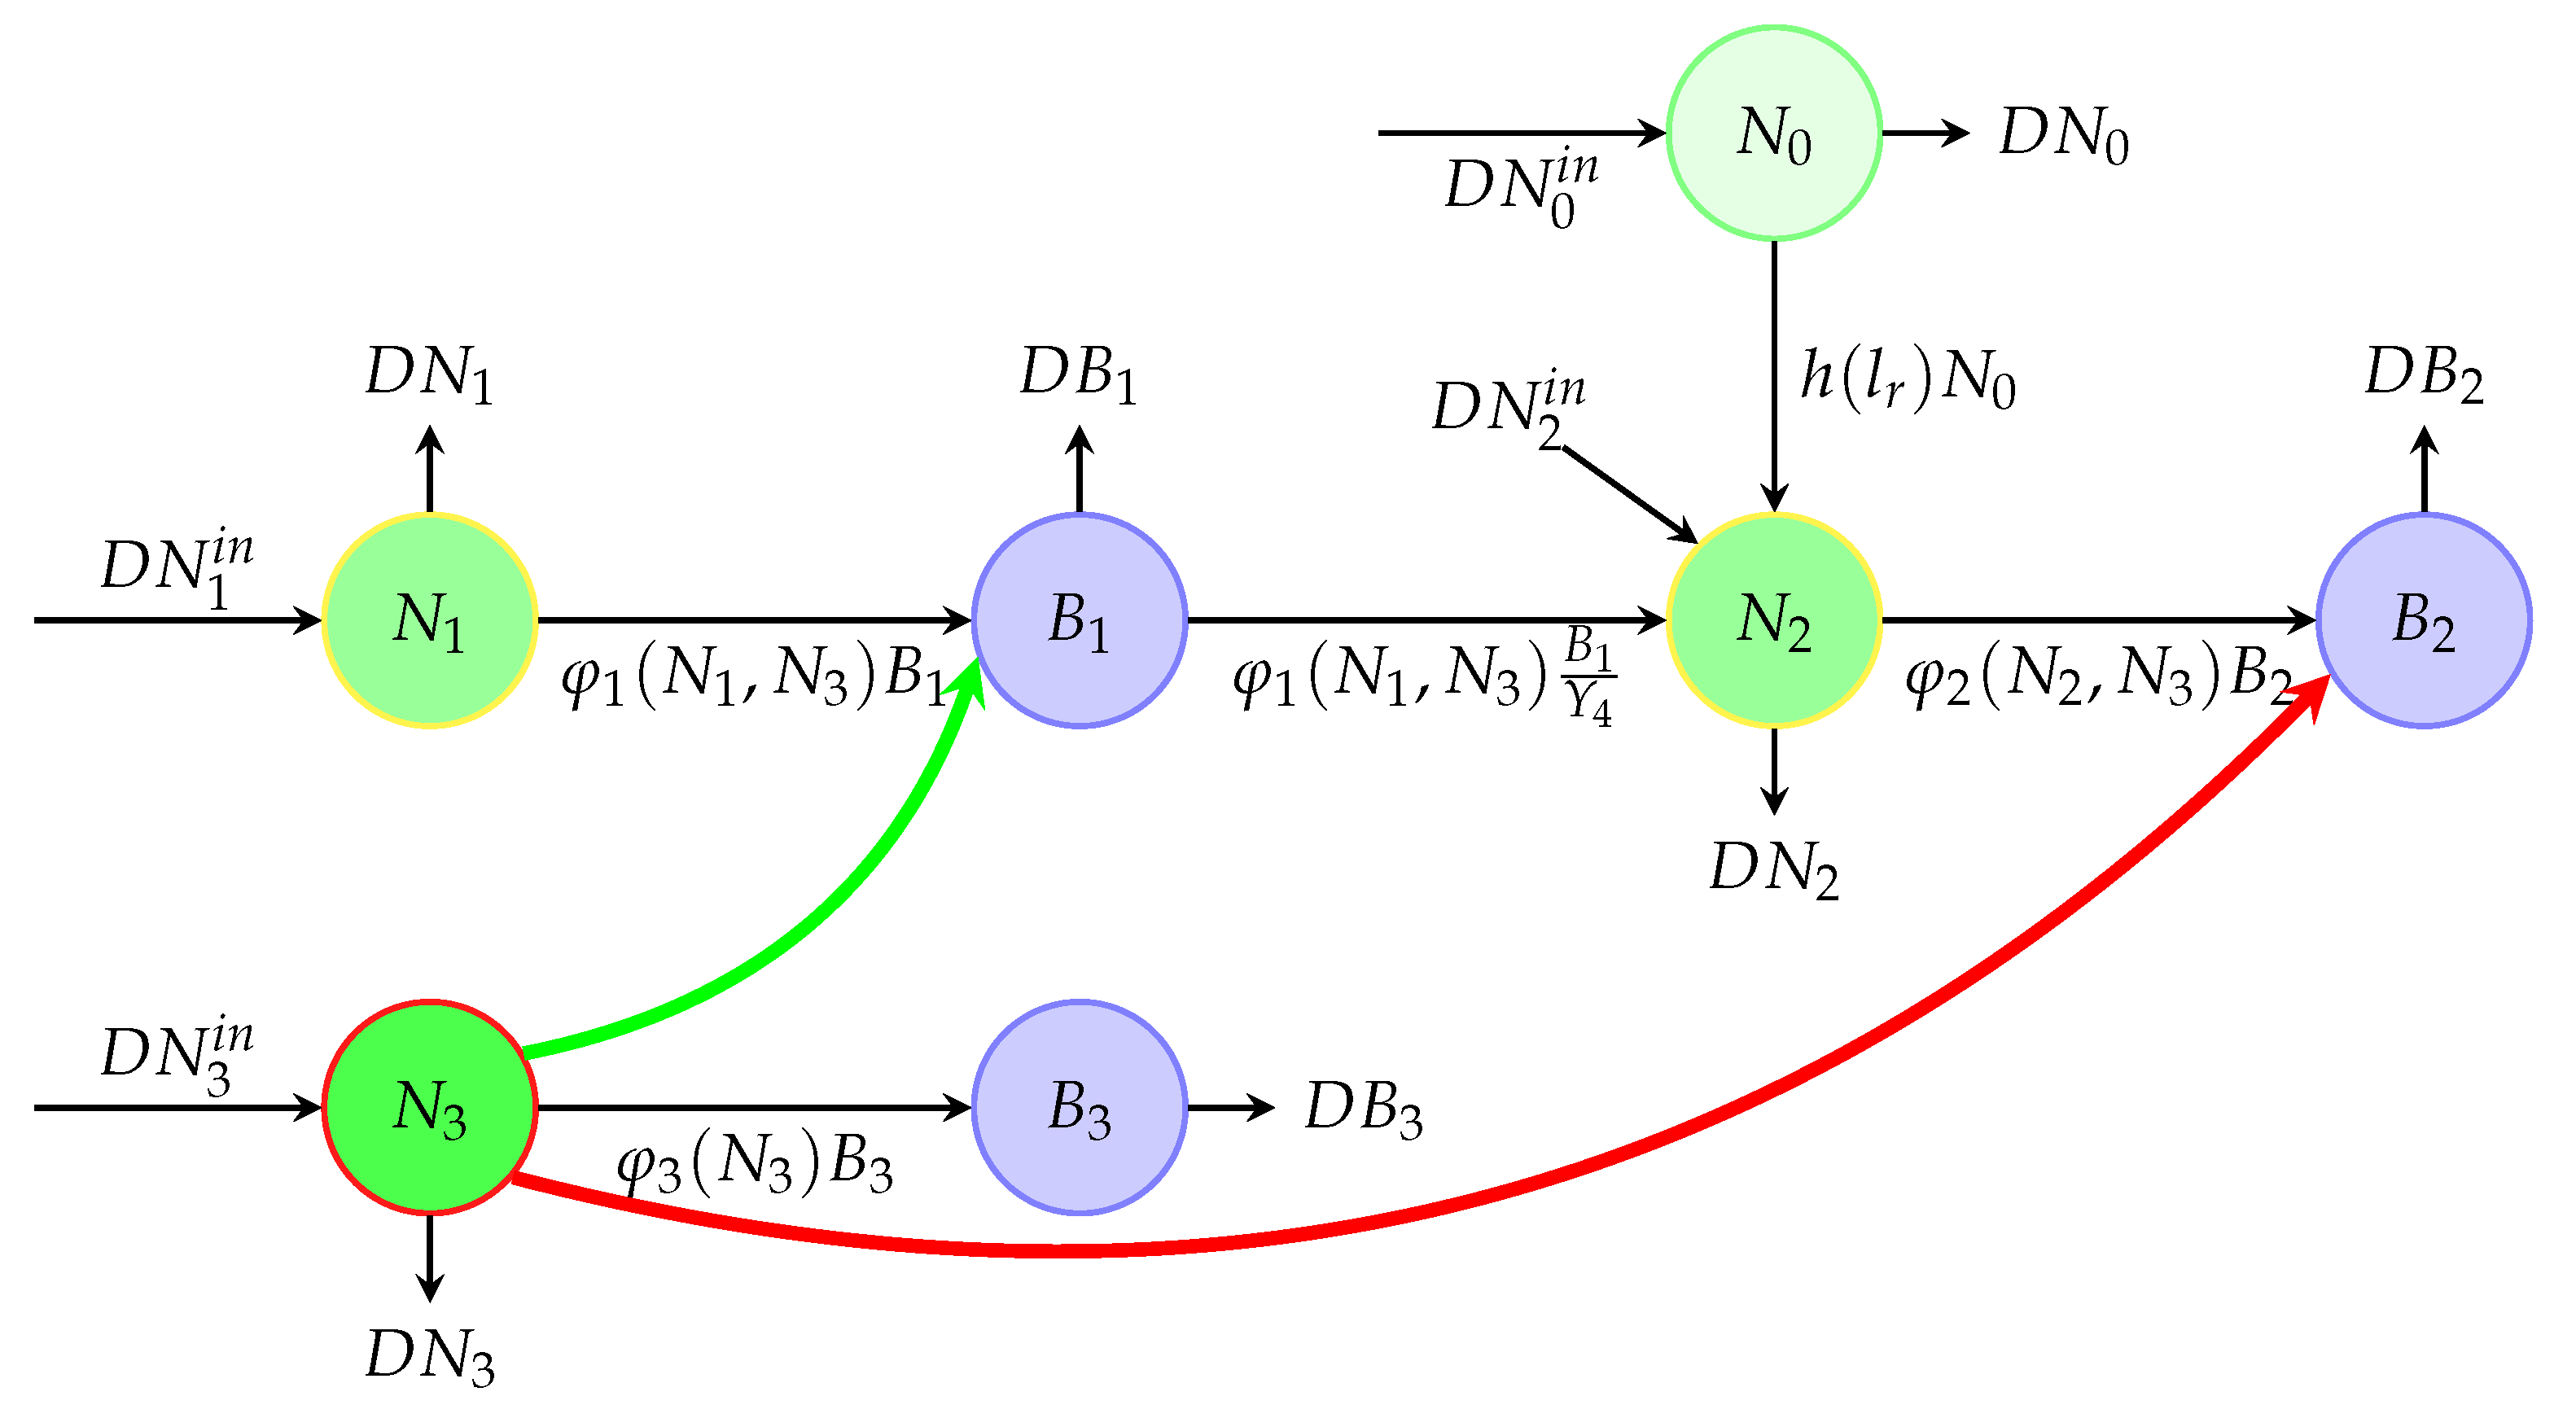
Anaerobic digestion Model No. 1 (ADM1) [8] serves as the foundation for the model created here. Three substrate and three biomass variables make up the basic model here, from which a sub-model characterizing phenol degradation and an extension of the entire model to include the extraneous substrates are produced and explained in the pertinent sections. The chlorophenol degrader produces phenol as a byproduct by using hydrogen and chlorophenol for growth. The phenol degrader grows on phenol to generate hydrogen, which also prevents it from growing. This hydrogen is scavenged by the methanogen, which serves as the main syntroph. Consider a chemostat (bioreactor, Figure 1) to which limiting substrates are continuously added (, , and ) where one of them is available in two forms (soluble and insoluble substrate; and ), while the culture liquid () is continuously mixed [9]. Both hydrogen () and chlorophenol () are used by the chlorophenol degrader () to grow, yielding phenol () as a byproduct. The hydrogen inhibits the phenol degrader (), which consumes phenol (). The methanogen () grows on the hydrogen (See Figure 2). The model that was suggested by Wade et al. [10] and examined by Sari and Wade [11] is revisited in the actual paper, taking into account two significant modifications that are pertinent from an applied standpoint. First, we solely consider the dilution rate and ignore all species-specific mortality (maintenance) rates. We disregard the portion of hydrogen generated by the phenol degrader in the second model update. Chlorophenol, phenol, and hydrogen are added to the chemostat at concentrations , respectively, and a constant dilution rate D.
Figure 1.
A continuous stirring reactor (chemostat) to which three limiting nutriments, where the first one of them is present in two forms (soluble and insoluble substrate; and ), are continuously added, while the culture liquid () is continuously mixed.
Figure 2.
Dynamics of three bacteria in a chemostat under the impact of the leachate recycling. Circles describe the compartments and [12,13].
Three biomass variables, four substrate variables, and seven components (Figure 2) make up the model created here, which is based on Anaerobic Digestion Model No. 1 (ADM1) (Batstone et al. [8]). Using hydrogen () and chlorophenol () for growth, the chlorophenol degrader () yields phenol in two forms: soluble () and insoluble (). The hydrogen inhibits the phenol degrader (), which consumes phenol (). The methanogen () grows on the hydrogen. The model suggested in [14] is revisited in the actual paper to take leachate recycling into account. The reactor is filled with leachate, chlorophenol, phenol, and hydrogen at a constant dilution rate D, leachate recirculation rate , and input concentrations , respectively. More details on the significance of the variables and parameters of the dynamics (1) and (2) are given in Table 1.
The following seven-dimensional dynamical system of ODEs is then used to represent the concentrations of species and substrates, providing a comprehensive framework for studying the complex interactions in a three-tiered microbial food web with leachate recirculation:
with initial value and yield parameters .
The three-tiered microbial food chain described by this suggested seven-dimensional dynamical model ignores maintenance in relation to the dilution rate. A complete stability study was undertaken both locally and globally in earlier investigations of two-tier ecological models [4,14,15].
To scale the system (2), the following adjustments to the parameters and variables are taken into account: , , , , , , , , , , . The dimensionless equations thus obtained are as follows:
Here, functions and are given by
Assume that the functional response of each species and satisfies:
Assumption 1.
- H1:
- and are of class
- H2:
- H3:
- H4:
- H5:
- and h are increasing functions.
Assumption H2 means that species cannot grow without substrates and and that the substrate is obligate for the growth of the biomass and that the nutriment is obligate for the growth of species . Hypothesis H3 expresses that the growth of species increases with the substrate and the substrate . Hypothesis H4 expresses that the species growth increases with the intermediate product produced by species . In contrast, the substrate inhibits . The growth of species rises with the substrate , according to hypothesis H5.
3. Preliminary Results
The steady states of the system (2), an appealing set, and some technical results will be presented in this section. These results will be used hereafter.
Lemma 1.
is the unique solution of
Lemma 2.
If the function satisfies Hypotheses H1, H2 and H3 and , then there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (4). □
Lemma 3.
If the function satisfies Hypotheses H1, H2 and H4 and ; then, there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (5). □
Lemma 4.
If the function satisfies Hypotheses H1, H2 and H5 and , then there exists a unique satisfying
Proof.
It is evident since , and is a continuous increasing function. □
Lemma 5.
If the function satisfies Hypotheses H1, H2 and H3 and , then there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (7). □
Lemma 6.
If the function satisfies Hypotheses H1, H2 and H4 and , then there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (8). □
Lemma 7.
If the function satisfies Hypotheses H1, H2 and H4 and , then there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (9). □
Lemma 8.
If the function satisfies Hypotheses H1, H2 and H4 and , then there exists a unique satisfying
Proof.
Let . It is easy to see that is a decreasing continuous function with and . Therefore, there exists a unique satisfying (10). □
Remark 1.
Let . By Hypotheses H1–H5, one can easily verify that:
We recall some basic features of the system (2) described on the non-negative cone (see, for example, [16]).
Proposition 1.
Proof.
- 1.
- To prove that the system (2) admits a unique solution, we apply the Cauchy–Lipschitz (Picard–Lindelöf) Theorem [17], which guarantees the existence and uniqueness of solutions to ordinary differential equations (ODEs) under Lipschitz continuity conditions. Let and express the system as:where is the vector field defined by the right-hand side of (2). By Assumption H1, the functions and h are . Since consists of sums, products, and compositions of functions, it follows that is also . A function on an open domain is locally Lipschitz continuous (by the mean value theorem). Because is open, is locally Lipschitz in . The fact that demonstrates the solution’s positive is:If then for and if then for .Now, if then .The next step is to demonstrate that the trajectories of (2) are bounded. Combining the system’s second and third equations yields, for , to a single equation:thenSimilarly, combining the system’s second and two last equations yields, for , to a single equation:thenFinally, combining the system’s first and the last four equations yields, for , to a single equation:thenwhere . The trajectory is bounded since every term in the three sums is positive. Thus, solutions remain bounded, and no finite-time blow-up occurs. By the Cauchy–Lipschitz Theorem, system (2) has a unique solution for all given initial conditions in .
- 2.
□
4. Reduction to a Third Dimensional Dynamics
Lemma 9.
Proof.
The prove of Lemma 9 is evident and it is omitted. □
Our goal is to investigate the asymptotic behavior of the seven-dimensional dynamics (14)–(15) trajectories, which converge exponentially inside the set . The goal is to limit the analysis of the system (14)–(15)’s asymptotic behavior to the attractive set . As a result, the reduced system’s asymptotic behavior will provide information about the full system (14)–(15). Keep in mind that periodic orbits are not disregarded in our situation.
The following reduced system provides the projection of the limitation of system (14)–(15) on in the space .
Since we proved previously that , then the projection of the system (14)-(15) on in the space leads to , and . Thus, for (16) the solution lies in the set given by:
4.1. Local Analysis
4.1.1. Steady States
The dynamics (16) admits the following possible eight steady states.
- Trivial steady state .
- Boundary steady states: , , , , and .
- Positive steady state .
4.1.2. Existence and Uniqueness
The existence and uniqueness conditions for each of the equilibrium points and , are given in the following theorem according to Lemmas 1–7.
Theorem 1.
- The existence and uniqueness of the steady state is always satisfied.
- The existence and uniqueness of the steady state is satisfied if and only if .
- The existence and uniqueness of the steady state is satisfied if and only if
- The existence and uniqueness of the steady state is satisfied if and only if .
- The existence and uniqueness of the steady state is satisfied if and only if .
- The existence and uniqueness of the steady state is satisfied if and only if .
- The existence and uniqueness of the steady state is satisfied if and only if .
- The existence and uniqueness of the steady state is satisfied if and only if .
Proof.
- exists always.
- The mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 2. Therefore, the existence and uniqueness of if and only if .
- The mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 3. Therefore, the existence and uniqueness of if and only if
- The mapping is increasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 4. Therefore, the existence and uniqueness of if and only if .
- exists if and only if . The mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 5. Therefore, the existence and uniqueness of if and only if .
- Similarly, the mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 6. Therefore, the existence and uniqueness of if and only if .
- exists and is unique if and only if according to Lemma 2. For , the mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 8. Therefore, the existence and uniqueness of if and only if .
- exists and is unique if and only if according to Lemma 4. exists and is unique if and only if according to Lemma 5. For , the mapping is decreasing. Therefore, the existence and uniqueness of such that if and only if according to Lemma 7. Therefore, the existence and uniqueness of if and only if .
□
4.1.3. Local Stability
The Jacobian matrix J of (16), at a point , is given by:
where the function is evaluated at , is evaluated at and is evaluated at . In the following lemma, the nature of the equilibrium point is given.
Lemma 10.
If then is a stable node. If then is an unstable node.
Proof.
The Jacobian matrix at is given by:
The eigenvalues are given by and . Thus, if then is stable. If , then is an unstable node. □
The nature of the boundary steady states , , , , , and is provided in the following lemmas.
Lemma 11.
is stable if . is an unstable node if .
Proof.
The Jacobian matrix at is given by:
where is evaluated at . The eigenvalues are given by
Thus, is stable if and it is unstable if . □
Lemma 12.
is stable if . It is unstable if .
Proof.
The Jacobian matrix at is given by:
where the function is evaluated at . The eigenvalues are
Thus, is stable if . It is unstable if . □
Lemma 13.
is stable if . is unstable if .
Proof.
The Jacobian matrix at is given by:
The eigenvalues are
Thus, is stable if . is unstable if . □
Lemma 14.
is stable if . is unstable if .
Proof.
The Jacobian matrix at is given by:
where the function is evaluated at , is evaluated at . Then, the eigenvalues are given by , and . Thus, is stable if . is unstable if □
Lemma 15.
The equilibrium point is stable if . is unstable if .
Proof.
The Jacobian matrix at is:
where the function is evaluated at and is evaluated at .
The characteristic polynomial is given by:
The eigenvalues are then given by as well as, according to Routh’s Stability Criterion, two additional negative eigenvalues. Therefore, the steady state is stable if ; however, it is unstable if . □
Lemma 16.
The steady state is stable if and it is unstable if .
Proof.
The Jacobian at is:
where the function is evaluated at .
The eigenvalues are given by
Therefore, the steady state is stable if and it is unstable if . □
Now, let us talk about the positive equilibria’s local stability.
Lemma 17.
The positive steady state is always stable.
Proof.
The Jacobian at is:
where the function is evaluated at and is evaluated at .
The Jacobian admits an eigenvalue given by and two other eigenvalues of the sub-matrix
It is clear that trace and det . Therefore, the positive steady state is always stable. □
The Table 2 provides a summary of the condition of existence, uniqueness, and nature of the steady states.
Table 2.
Existence, uniqueness, and steady states’ nature.
4.2. Global Analysis
In the following, we solely take into account the interesting situation where
- H6:
Hypothesis H6 guarantees that ; therefore, is the only stable steady state for the dynamics (16). , , , , , and are unstable steady states.
Remark 2.
Consider the dynamics (16) solution that is a part of . Let us examine how the variables , change to transform the system (16). The new dynamics that follows is thus obtained:
We have
The dynamics (17) has no invariant sets (including tori) with no-zero volume that are entirely in Ω, according to the Dulac criterion [16]. It must be a fractal set with zero volume if there is an odd attractor. Note that periodic orbits (of zeros volume) are not excluded.
- . According to the Dulac criterion [16], the dynamics (16) has no periodic solution inside the face ().
- . According to the Dulac criterion [16], the dynamics (16) has no periodic solution inside the face ().
- . According to the Dulac criterion [16], the dynamics (16) has no periodic solution inside the face ().
Lemma 18.
(Butler–McGehee Lemma [16]) Consider to be a continuously differentiable function. Let to be a hyperbolic equilibrium of the dynamics with . Let to be the positive semi-orbit through and to be the omega limit set of . Assume that is in , but is not the entire omega limit set. Then, admits a non-trivial intersection with both stable and unstable manifolds of .
Theorem 2.
For every initial conditions in , the three bacteria persist, i.e.,
Proof.
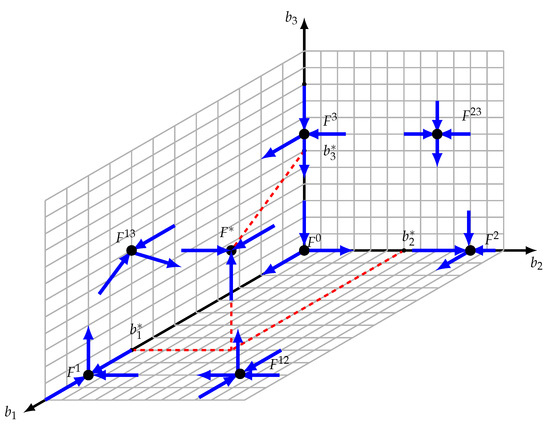
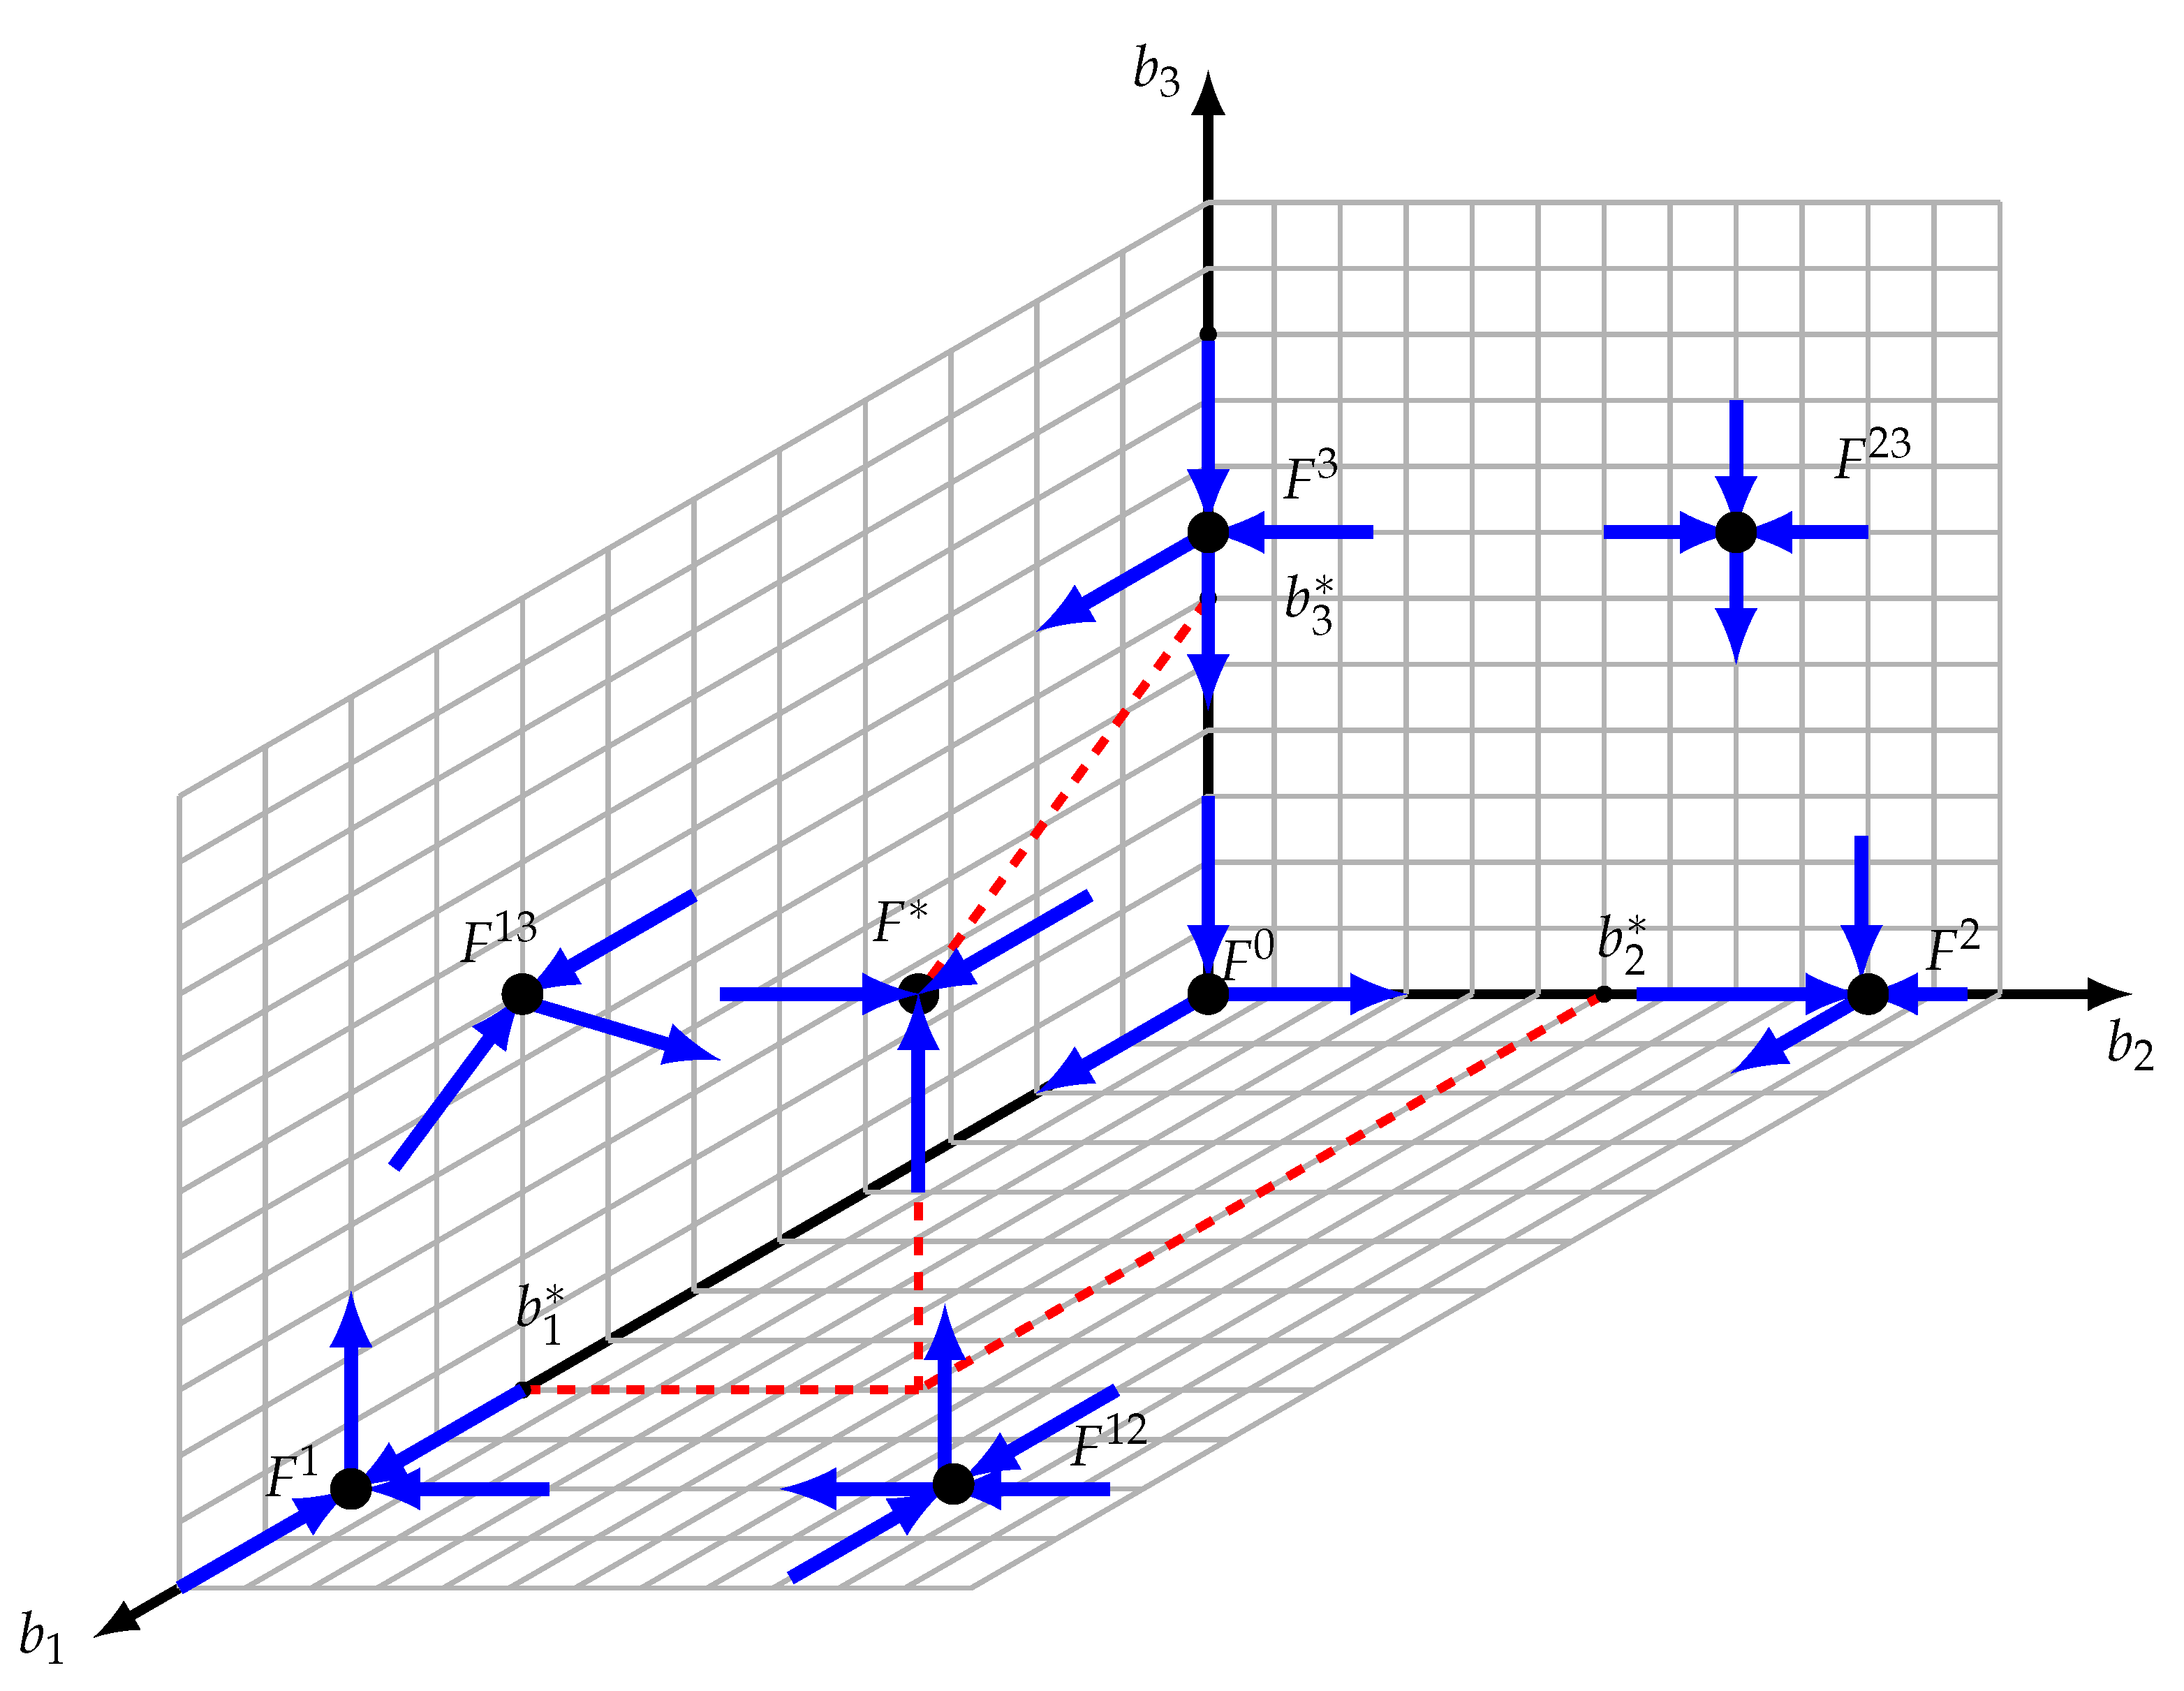
The goal of this proof is to demonstrate the three species’ cohabitation using the model’s uniform persistence (16). The system’s boundary equilibria (16) are all unstable in our scenario. Let and the omega limit set of , which is compact and invariant such that . The stable and unstable manifolds of the border equilibria are known and displayed in Figure 3 to simplify the argument because the faces , , and are invariant. Assume that a point Z on the edge of the positive cone is contained in and let be the positive semi-orbit through Z. Therefore,
Figure 3.
Equilibria configuration. , , , , , , and are unstable steady states, and is the only stable one.
- Because is unstable could not be a part of the omega limit set of , and thus Z cannot be .
- If (similarly, or ). Since is invariant, thus will be a subset of and this is not possible because is bounded and (similarly, or ).
- If (similarly, or ). contains (similarly, or ). Since is a compact, then it includes (similarly, or ). In particular, contains , which is not possible.
- If (similarly, or ). is not reduced to (similarly to or to ). According to the Theorem of Butler–McGehee, includes a point Q of different than (similarly, of different than or different than ) and this is impossible.
- If (similarly, or ). Since is invariant then and this is not possible as is bounded and (similarly, or ).
- If (similarly, or or or or ). Since is invariant then and this is not possible as is bounded and (similarly, or or or or ).
- If (similarly, or ). contains (similarly, or ). As is a compact, then it contains the adherence of , (similarly, or ). In particular, contains and this is impossible.
- If (similarly, or ). is not reduced to (similarly to or to ). According to the Theorem of Butler–McGehee, includes a point Q of other that (similarly, of other that or other that ) and this is impossible.
The omega limit set cannot contain any points on the positive cone ’s border. The ”positive” periodic orbit of system (16) may exist inside . The solution of the system (16) converges asymptotically to either the unique stable node or to a “positive” periodic orbit (if one exists) according to the Poincaré–Bendixon Theorem [16]. Therefore,
□
5. Back to
Theorem 3.
Assume that the dynamics (2) satisfies Assumptions H1 to H6 such that in , then the three bacteria persist which means that and .
Proof.
Hence, is a solution of the non-autonomous dynamics given hereafter:
Asymptotically, the dynamics (18) converges to the autonomous dynamics (16). The phase portrait of the reduced (to ) dynamics (16) shows just one locally stable node, and the other are unstable steady states, and a potential ”positive” periodic trajectory. Furthermore, is an attractor of all solutions in . According to Thiemes’s findings [18], it can be concluded that the asymptotic behavior of the trajectory of the dynamics (18) is identical to that of the reduced dynamics (16). After that, the outcome is inferred. □
We make the assumption for the remainder of the study that with is a constant.
6. Optimal Strategy
Leachate recirculation in a chemostat can be optimally controlled by dynamically modifying the recirculation rate to optimize bioreactor performance (e.g., waste degradation, biogas production) while reducing environmental impacts and operating costs. An organized method for defining and resolving this issue is provided below. Suppose that the leachate is continually fed to the chemostat at a rate that differs from the D dilution rate. The primary objective of the optimal strategy is to apply the initial control action and solve a finite-time optimal control problem at each stage in order to minimize the organic matter inside the reactor through a minimal rate of leachate recirculation. The rate (recirculation costs) will, therefore, be assumed to be variable on the interval , with . Suppose that , , and are globally Lipschitz functions with Lipschitz parameters, , , and , respectively, and maximums , and . Thus, we aim to find the optimal control function in the admissible set
that minimizes the following functional
For suitable constants and , our goal is to keep the control costs as low as possible while minimizing the amount of organic matter in its two forms. The existence of the optimal control and the associated state can be readily demonstrated by applying the theory in [19].
Theorem 4.
is uniformly Lipschitz.
Proof.
It is evident that , the continuous function, is uniformly Lipschitz since we have
where . The matrix B satisfies ; thus, with and thus, the continuous function, is uniformly Lipschitz. □
Therefore, there is only one solution to the dynamics (19). The control problem can be examined through the Hamiltonian function in the following way by applying Pontryagin’s Maximum principle [19,20,21]:
The adjoint unknowns , , , , , , and are solutions of the following adjoint system
satisfying , , , , , , and . The Hamiltonian’s derivatives are provided by
Therefore, admits a unique solution provided by
provided that and . Therefore, the control is characterized as follows:
7. Numerical Investigations
To demonstrate the accuracy of the theory derived above, a few examples are given below. The following functions are proposed to express the growth rates and the leachate re-circulation rate:
where , , , and are positive constants.
It is easy to see that the functions , , , and h satisfy Hypotheses H1–H5 where the parameters values are chosen as in Table 3.
Table 3.
The numerical simulations’ selected parameters have no biologically significant practical implications; they are merely intended to illustrate the findings.
7.1. Numerical Investigation for the Dynamics (2)
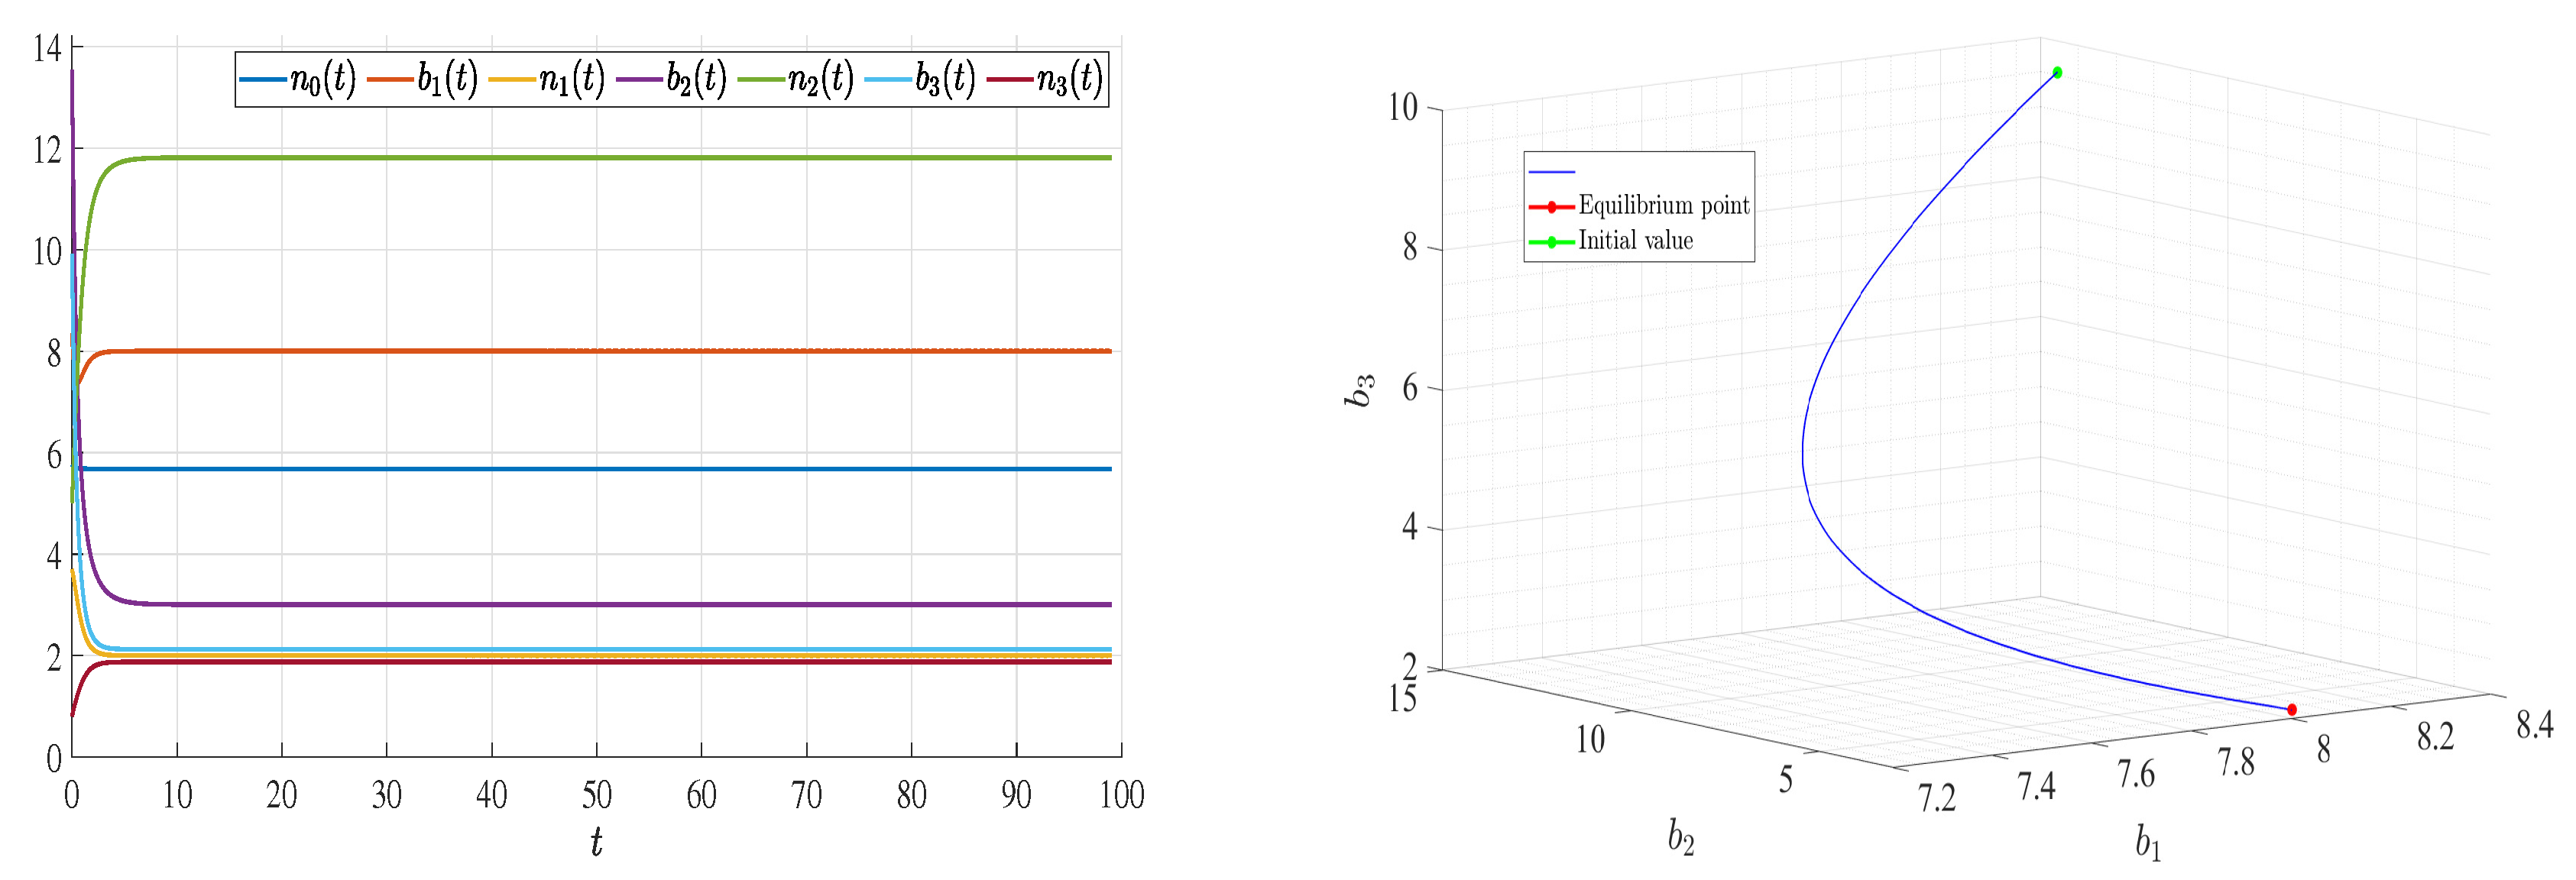
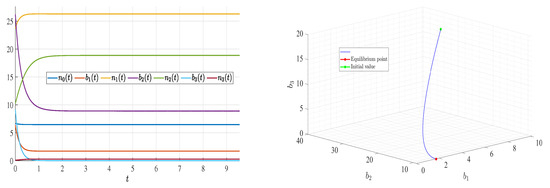
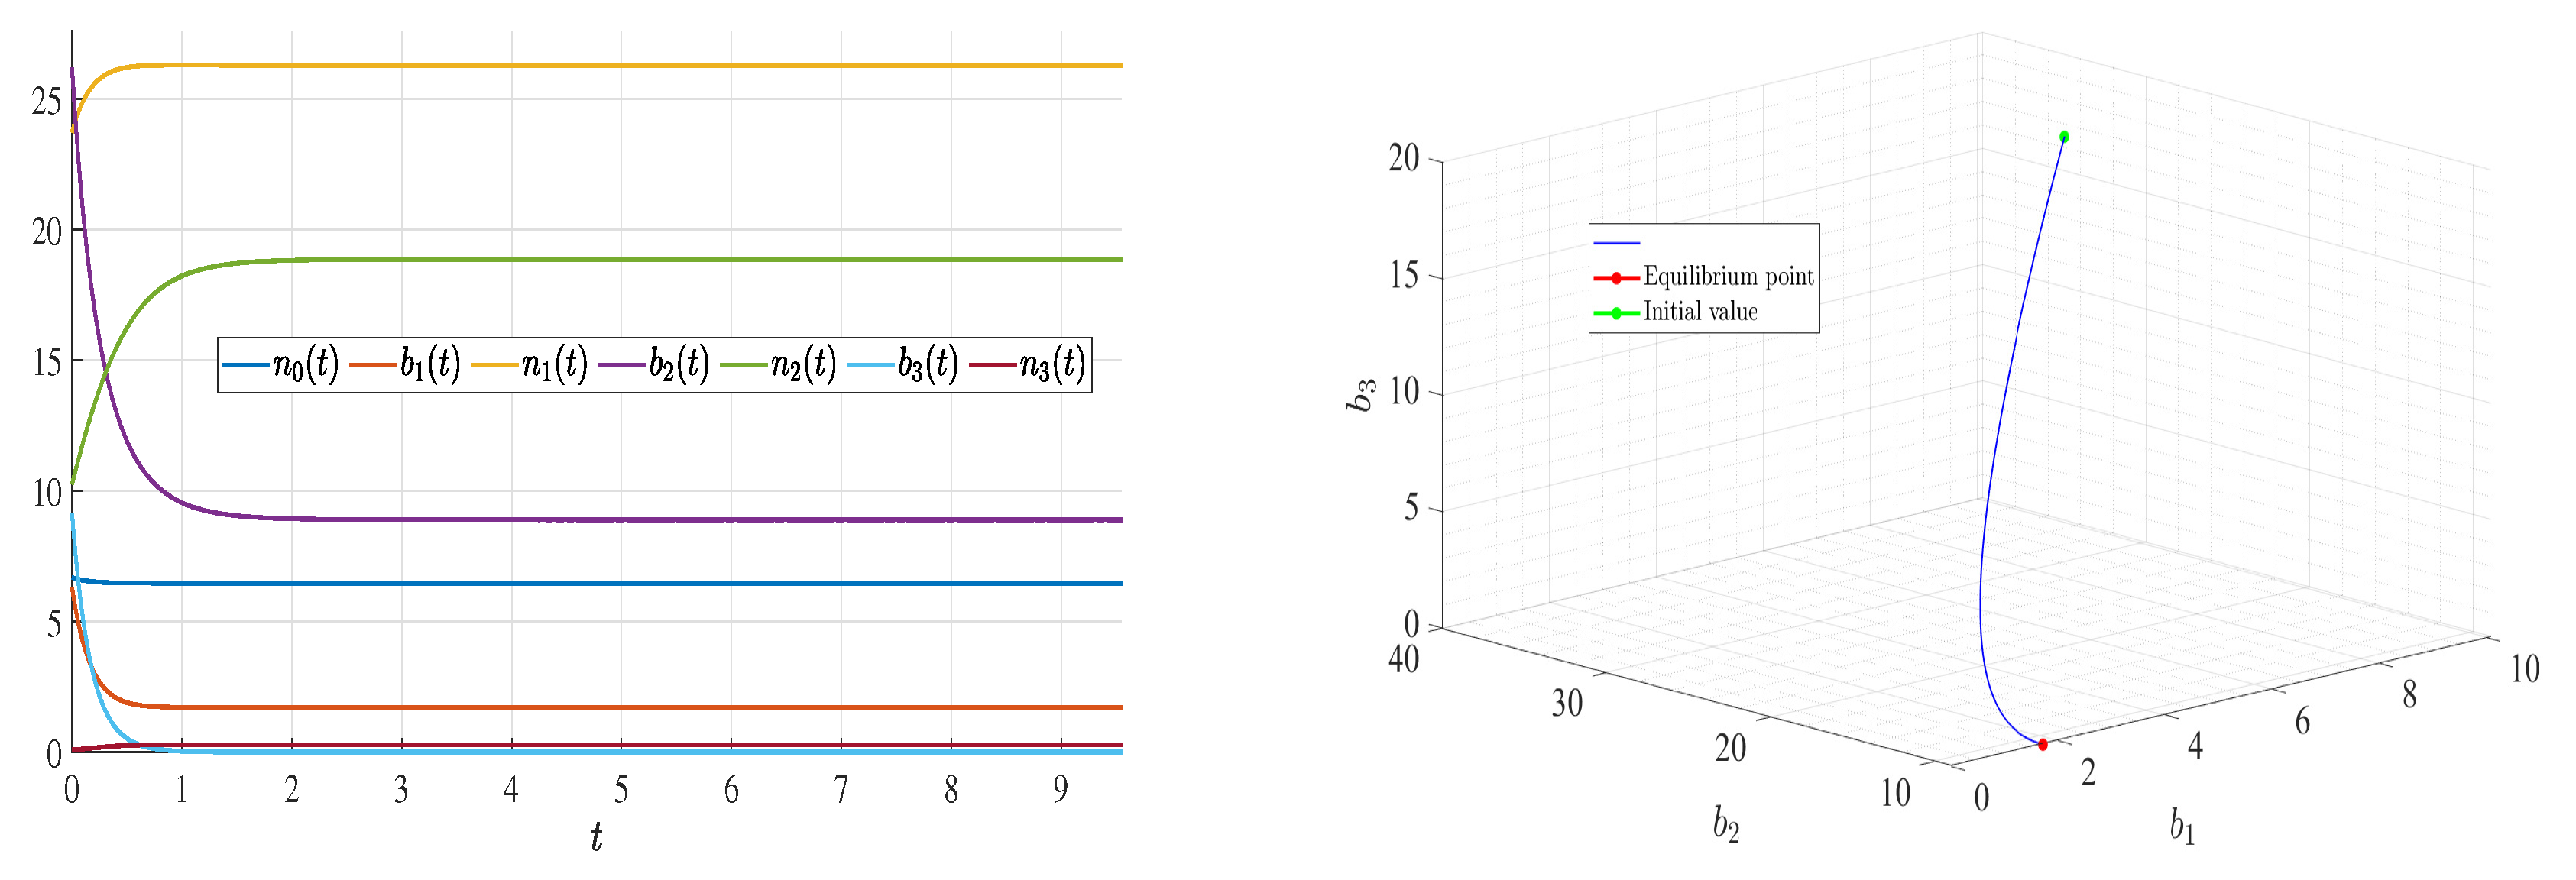
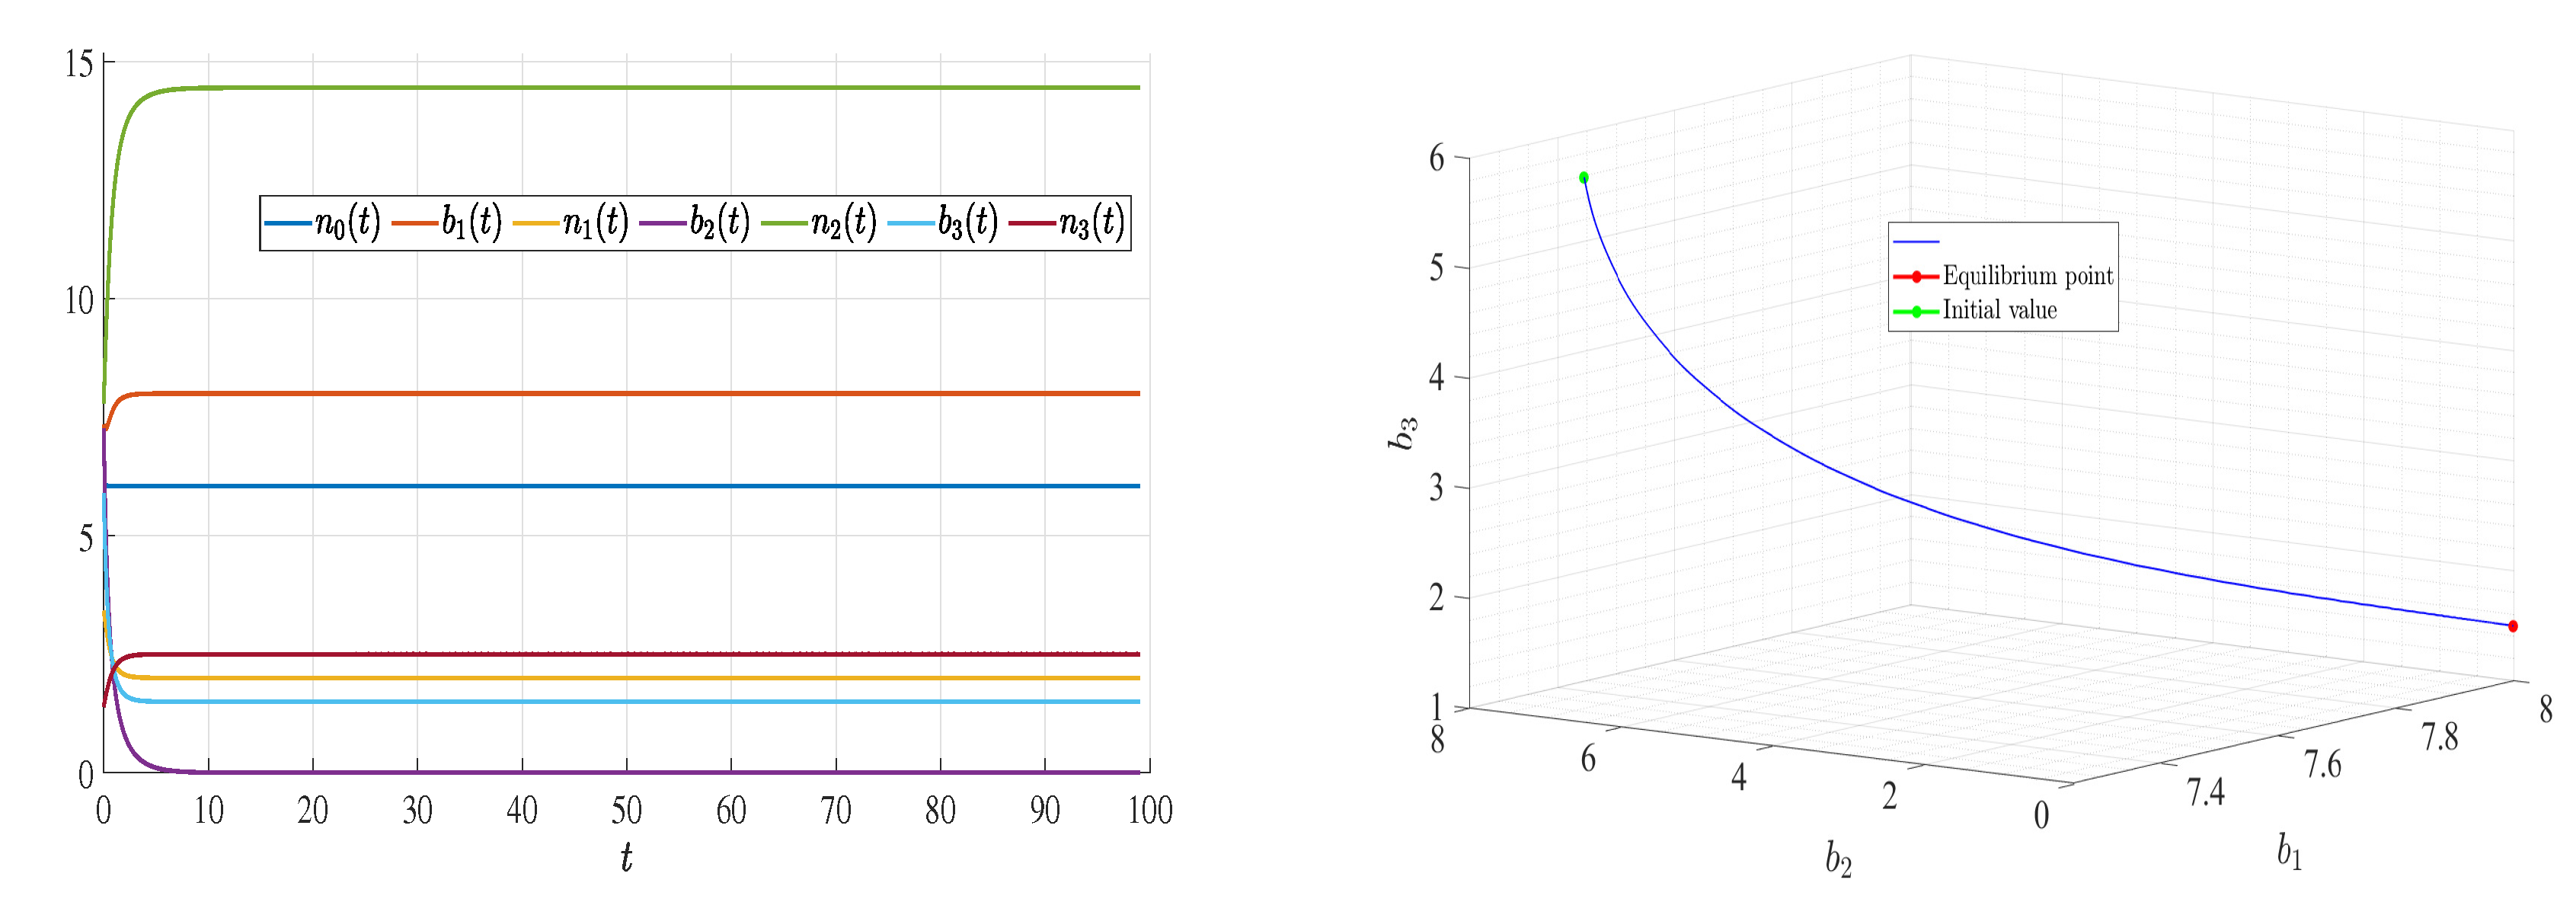
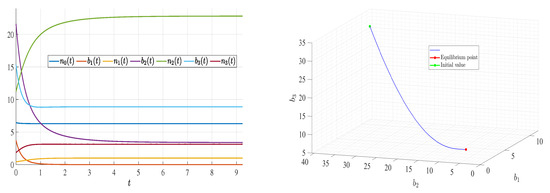
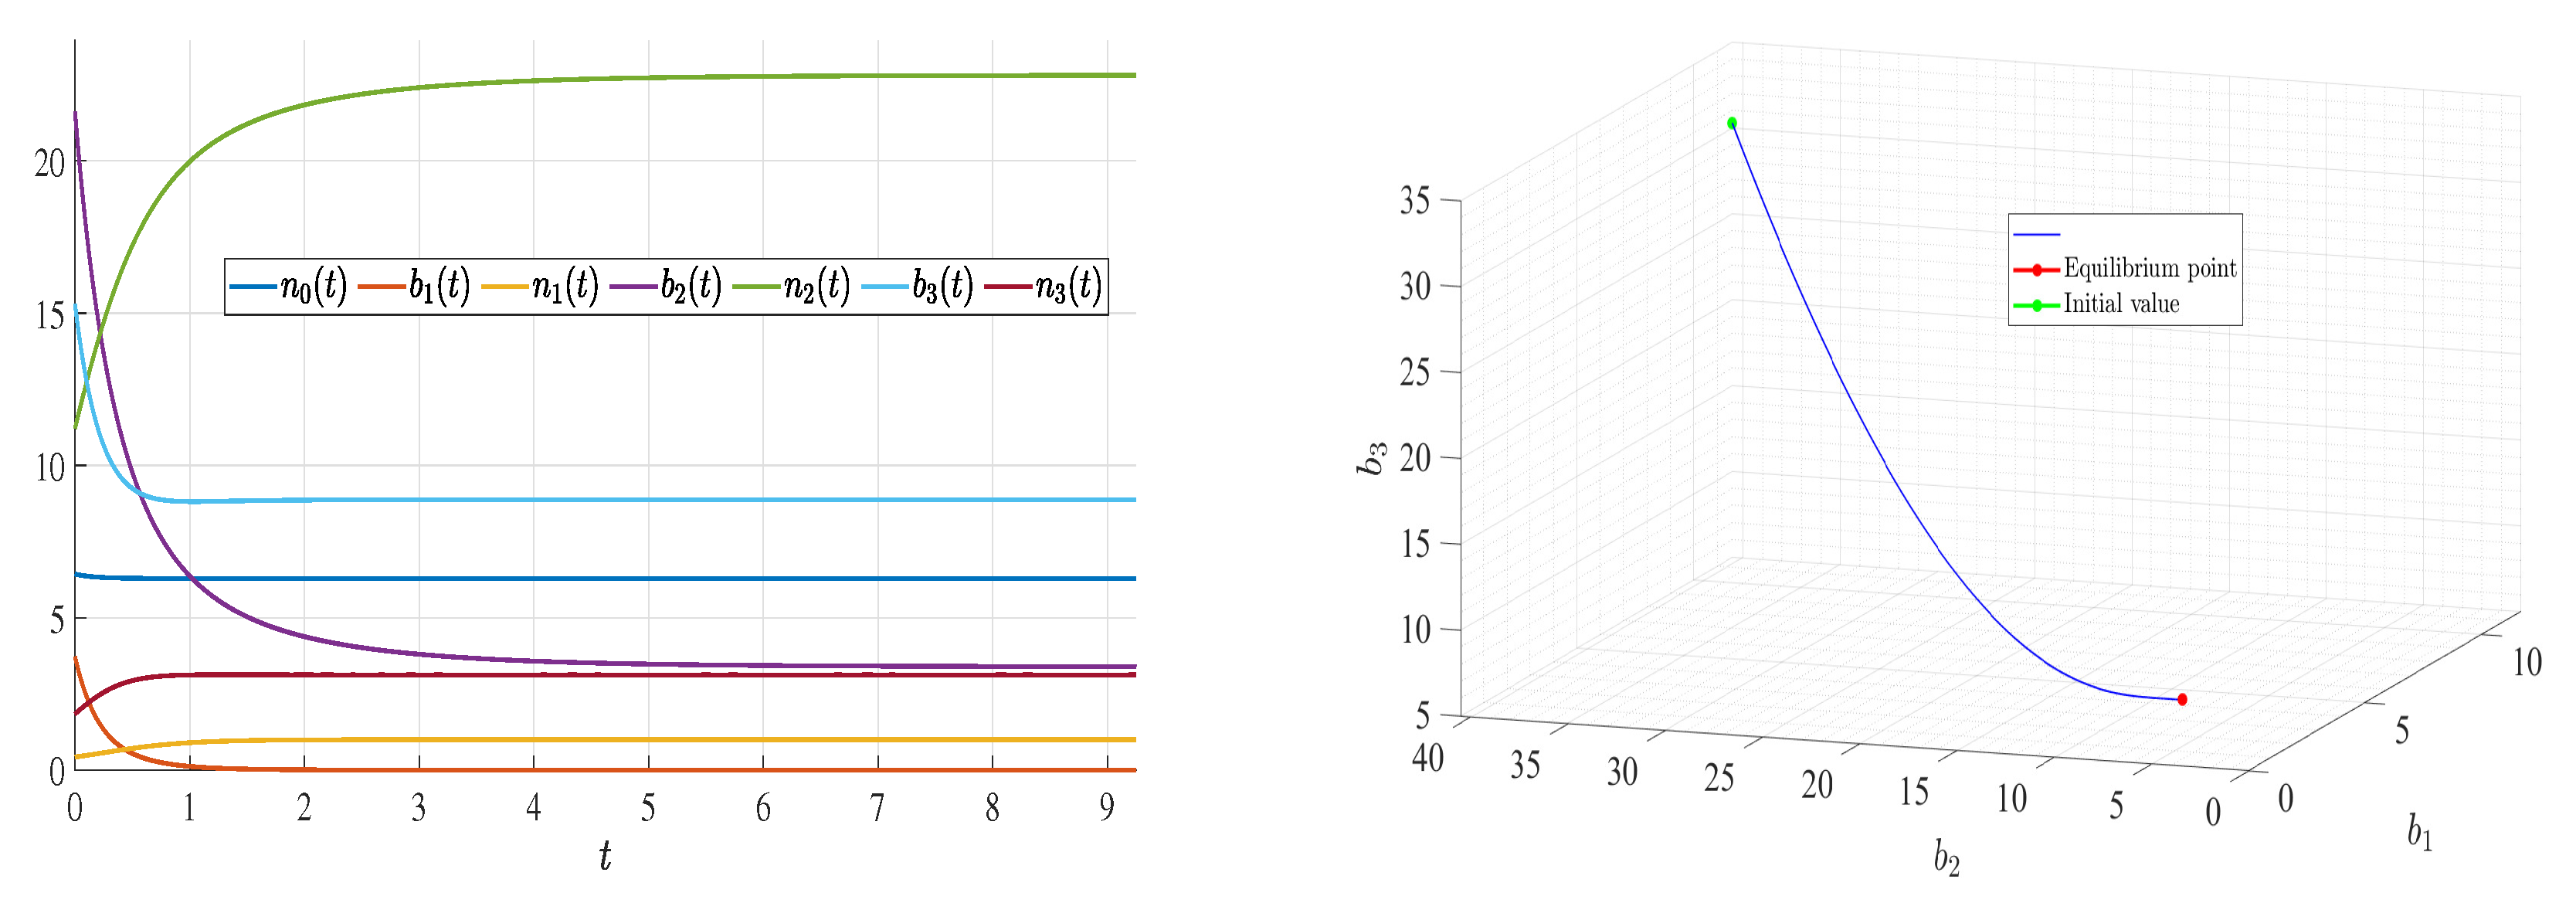
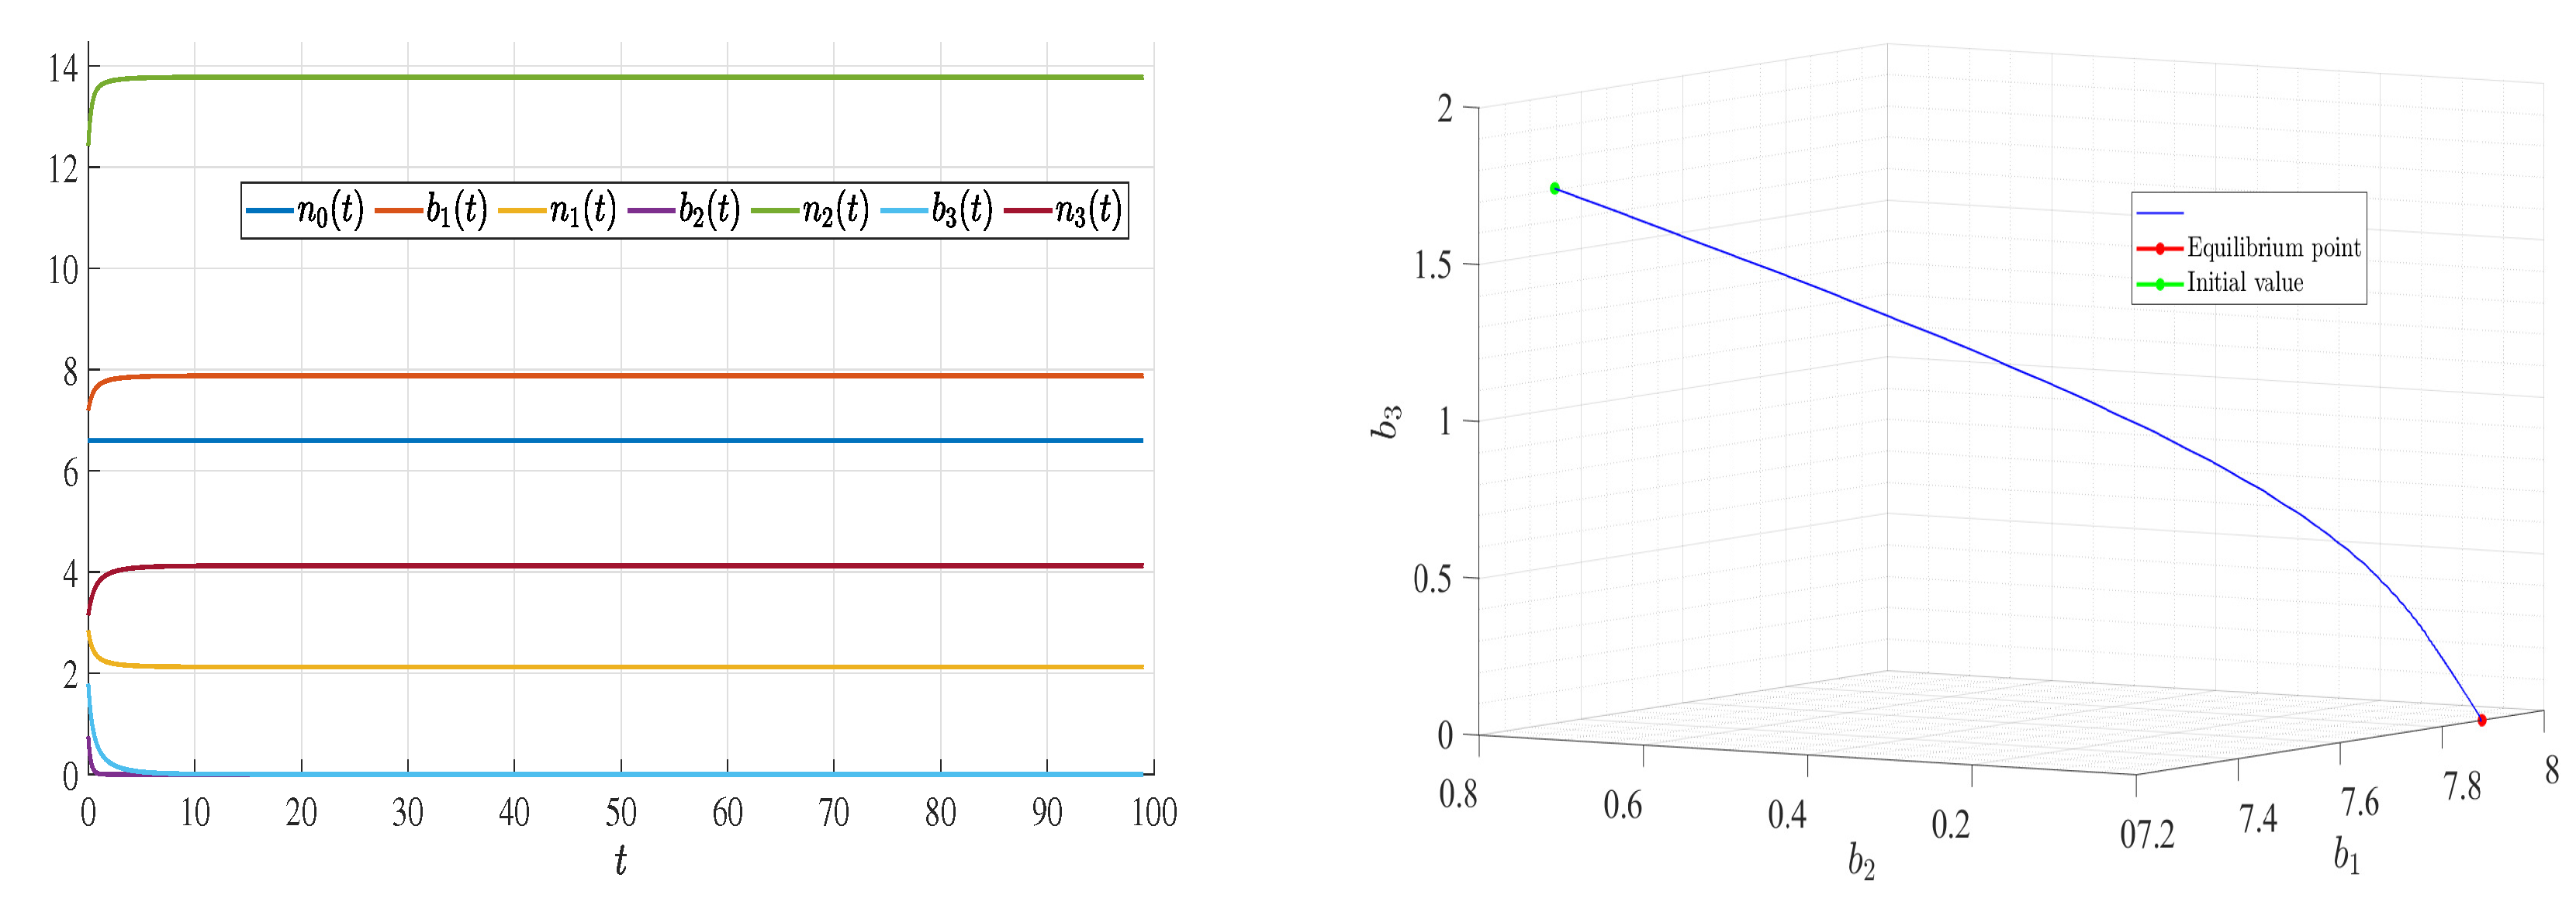
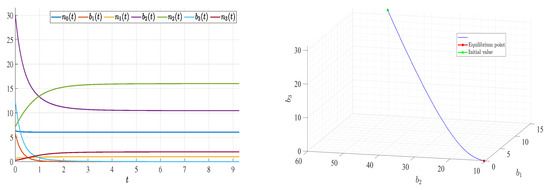
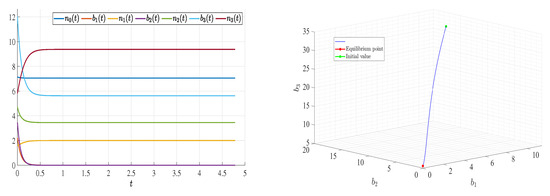
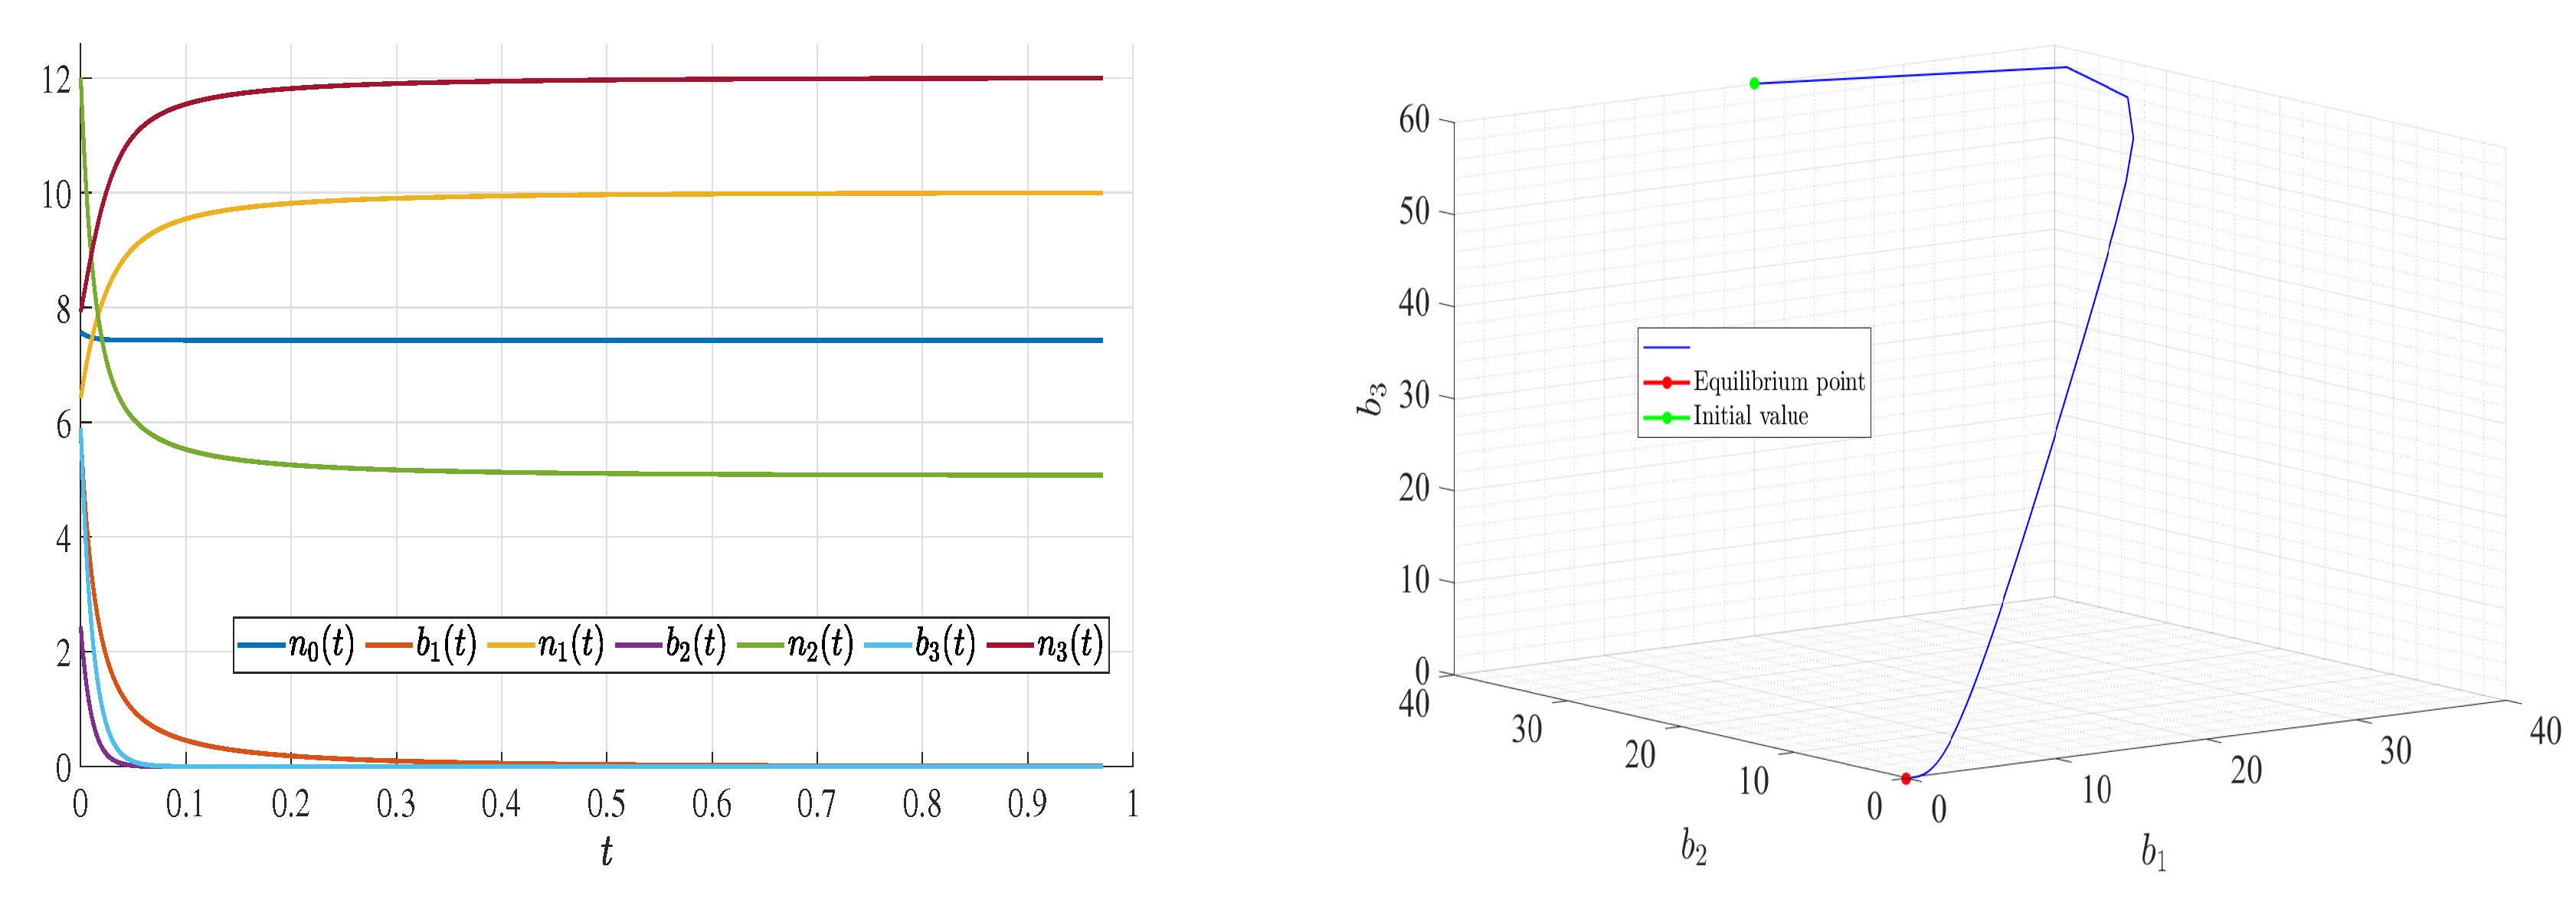
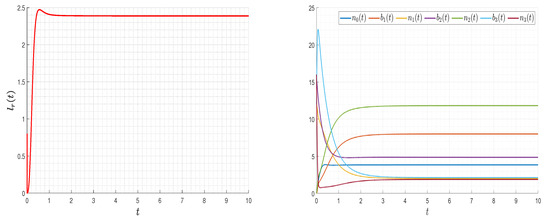
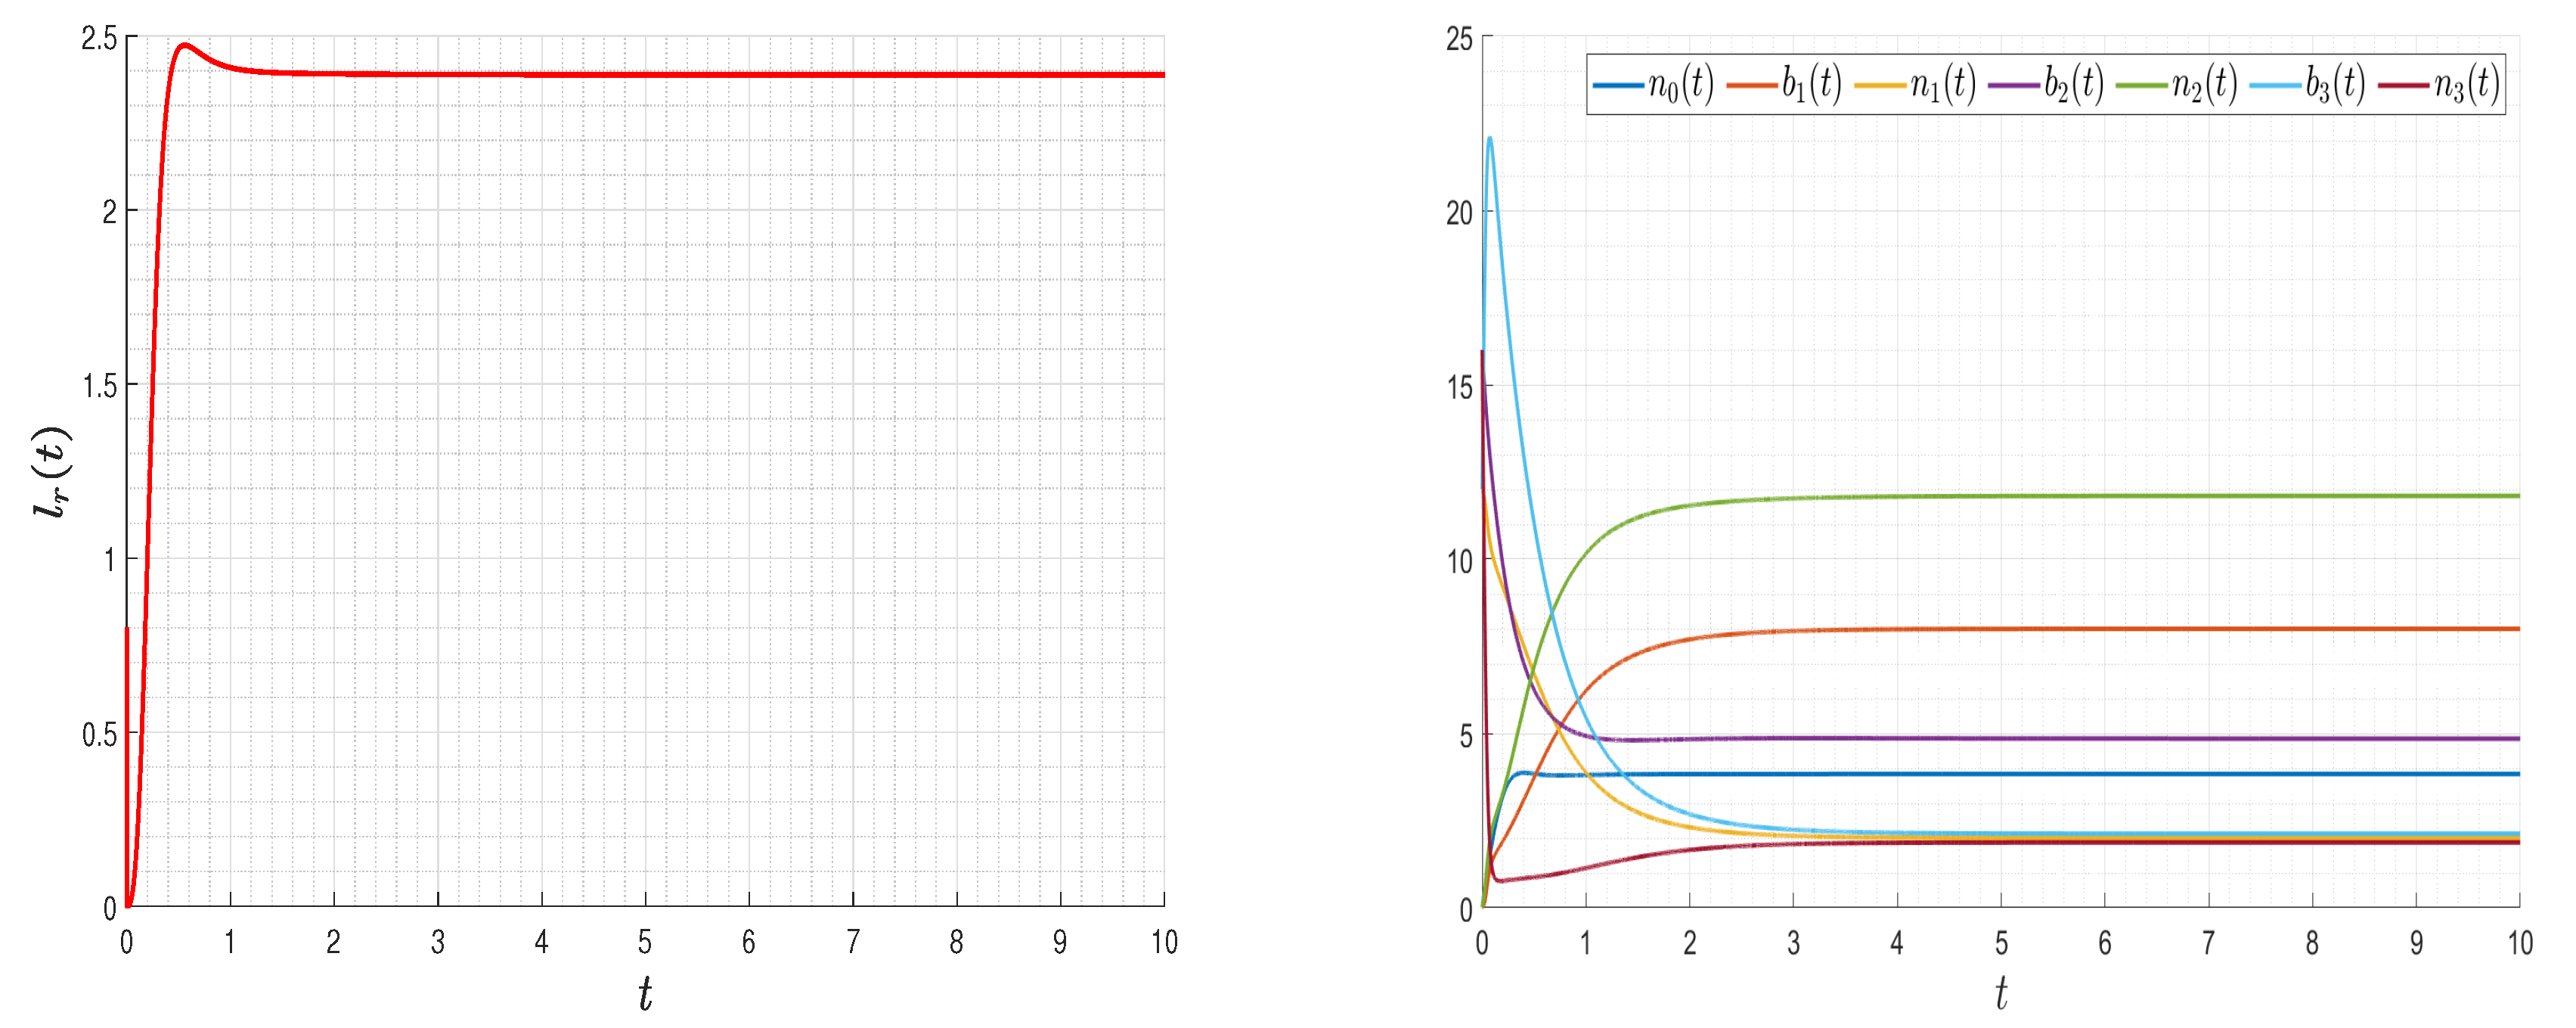
We start by solving the direct problem (2) numerically by choosing the leachate recirculation rate as . The first test satisfies H1 to H6 ensuring the global stability of the unique positive steady state . The persistence of competing bacteria can be seen in Figure 4. In Figure 5, the solution of (2) converges to the equilibrium , and only the two bacteria and persist. In Figure 6, the solution of (2) converges to the equilibrium , and only the two bacteria and persist. In Figure 7, the solution of (2) converges to the equilibrium , and only the two bacteria and persist. In Figure 8, the solution of (2) converges to the equilibrium , and only bacteria 1 persists. In Figure 9, the solution of (2) converges to the equilibrium , and only bacteria 2 persists. In Figure 10, the solution of (2) converges to the equilibrium , and only bacteria 3 persists. Finally, in Figure 11, the solution of (2) converges to the equilibrium , and all bacteria go extinct.
Figure 4.
For , , , and , the trajectory of dynamics (2) converges to , and all bacteria persist.
Figure 5.
For , , , and , the solution of (2) converges to , and only bacteria and persist.
Figure 6.
For , , , and , the solution of (2) converges to , and only bacteria and persist.
Figure 7.
For , , , and , the solution of (2) converges to , and only bacteria and persist.
Figure 8.
For , , , and , the solution of (2) converges to , and only bacteria persists.
Figure 9.
For , , , and , the solution of (2) converges to , and only bacteria persists.
Figure 10.
For , , , and , the solution of (2) converges to , and only bacteria persists.
Figure 11.
For , , , and , the solution of (2) converges to , and all bacteria go to extinction.
7.2. Numerical Investigation for the Optimal Control Problem
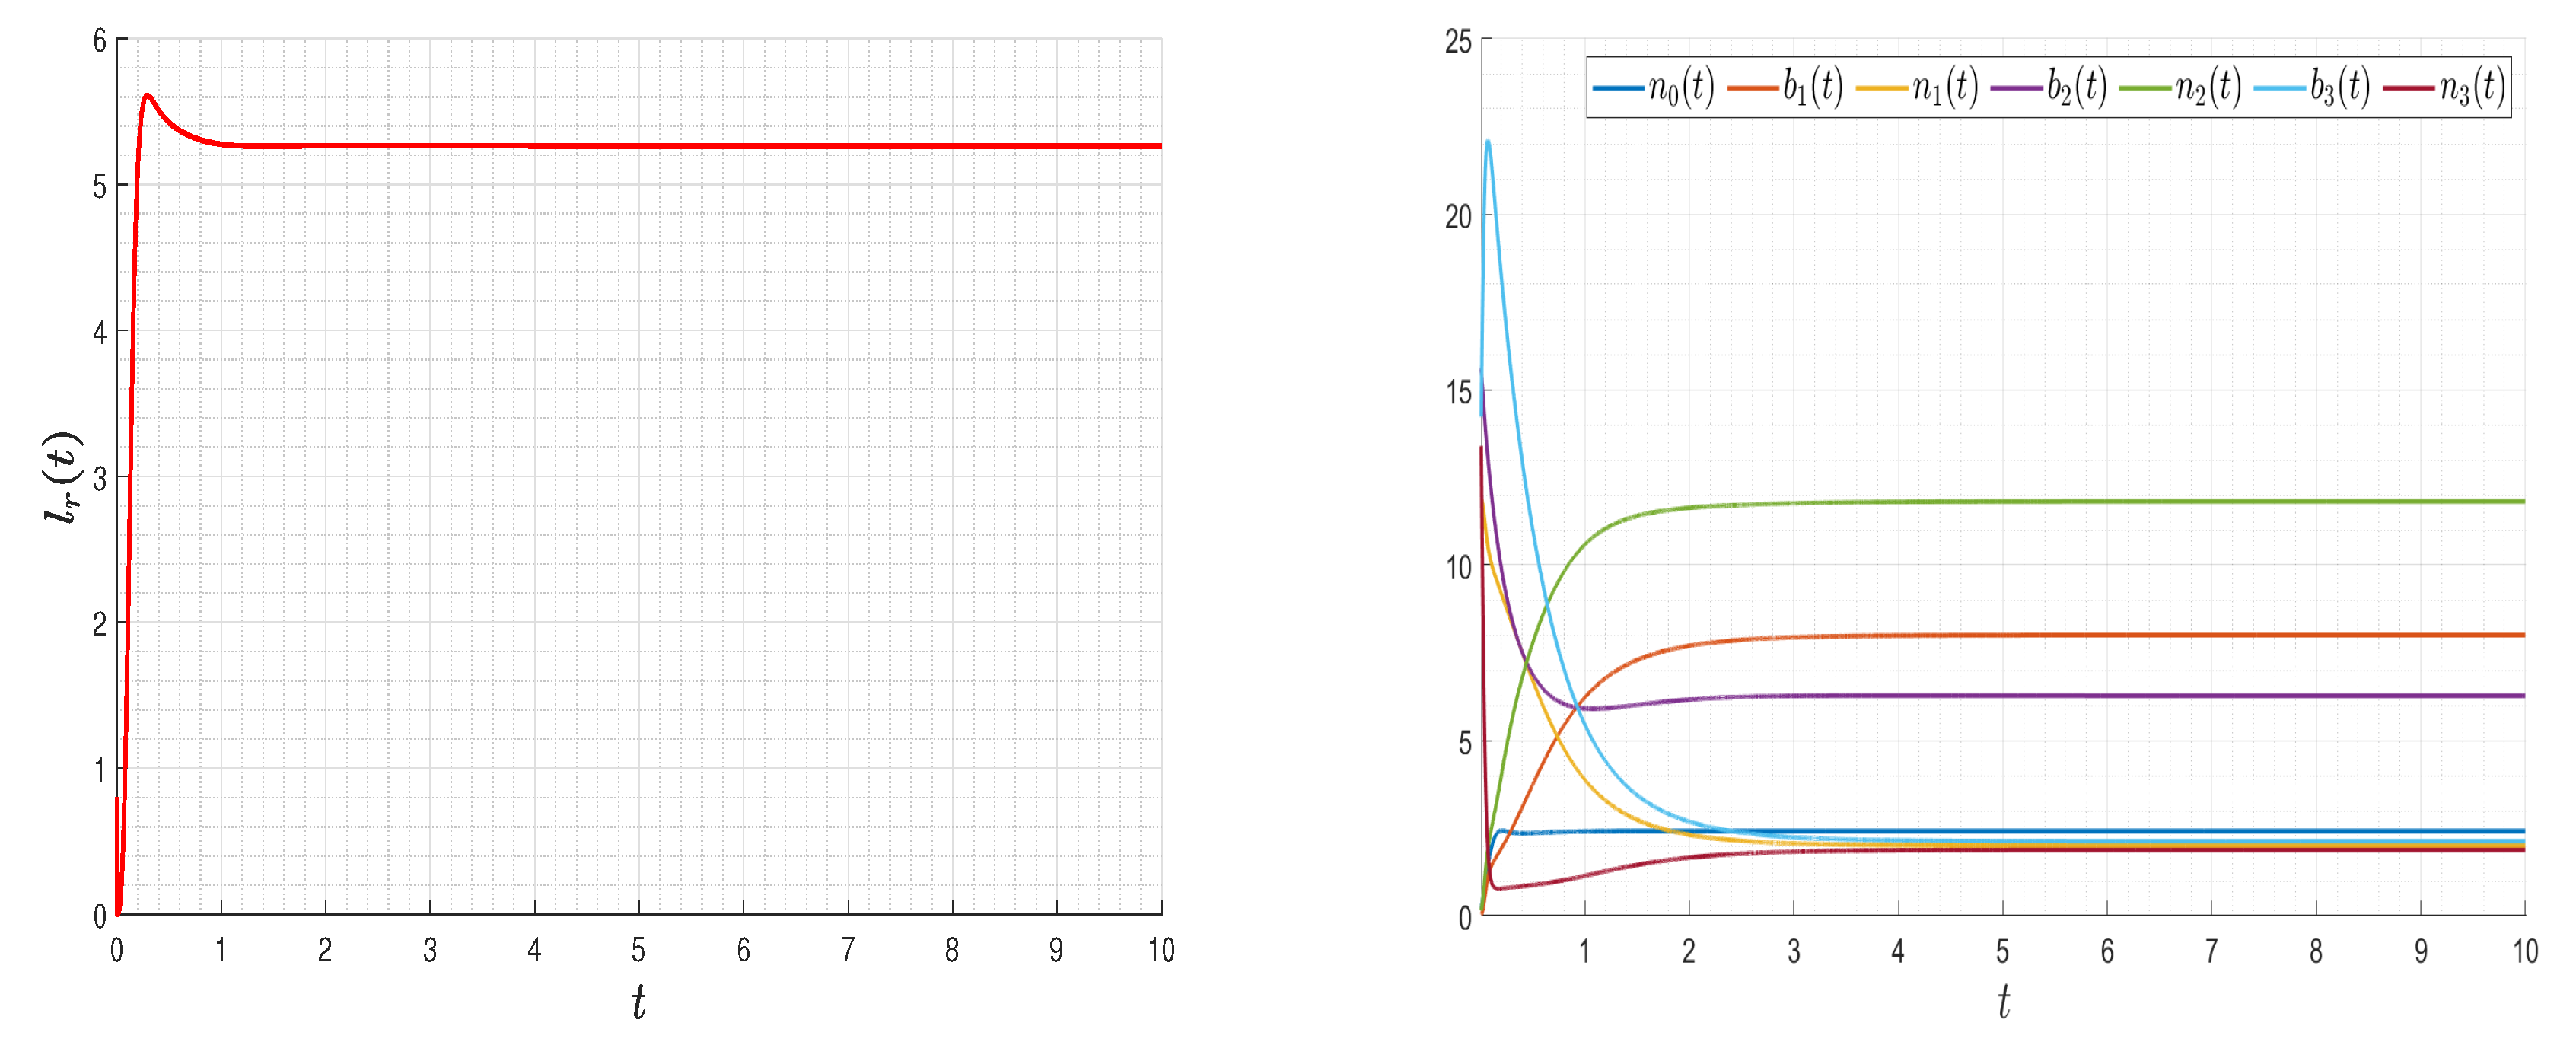
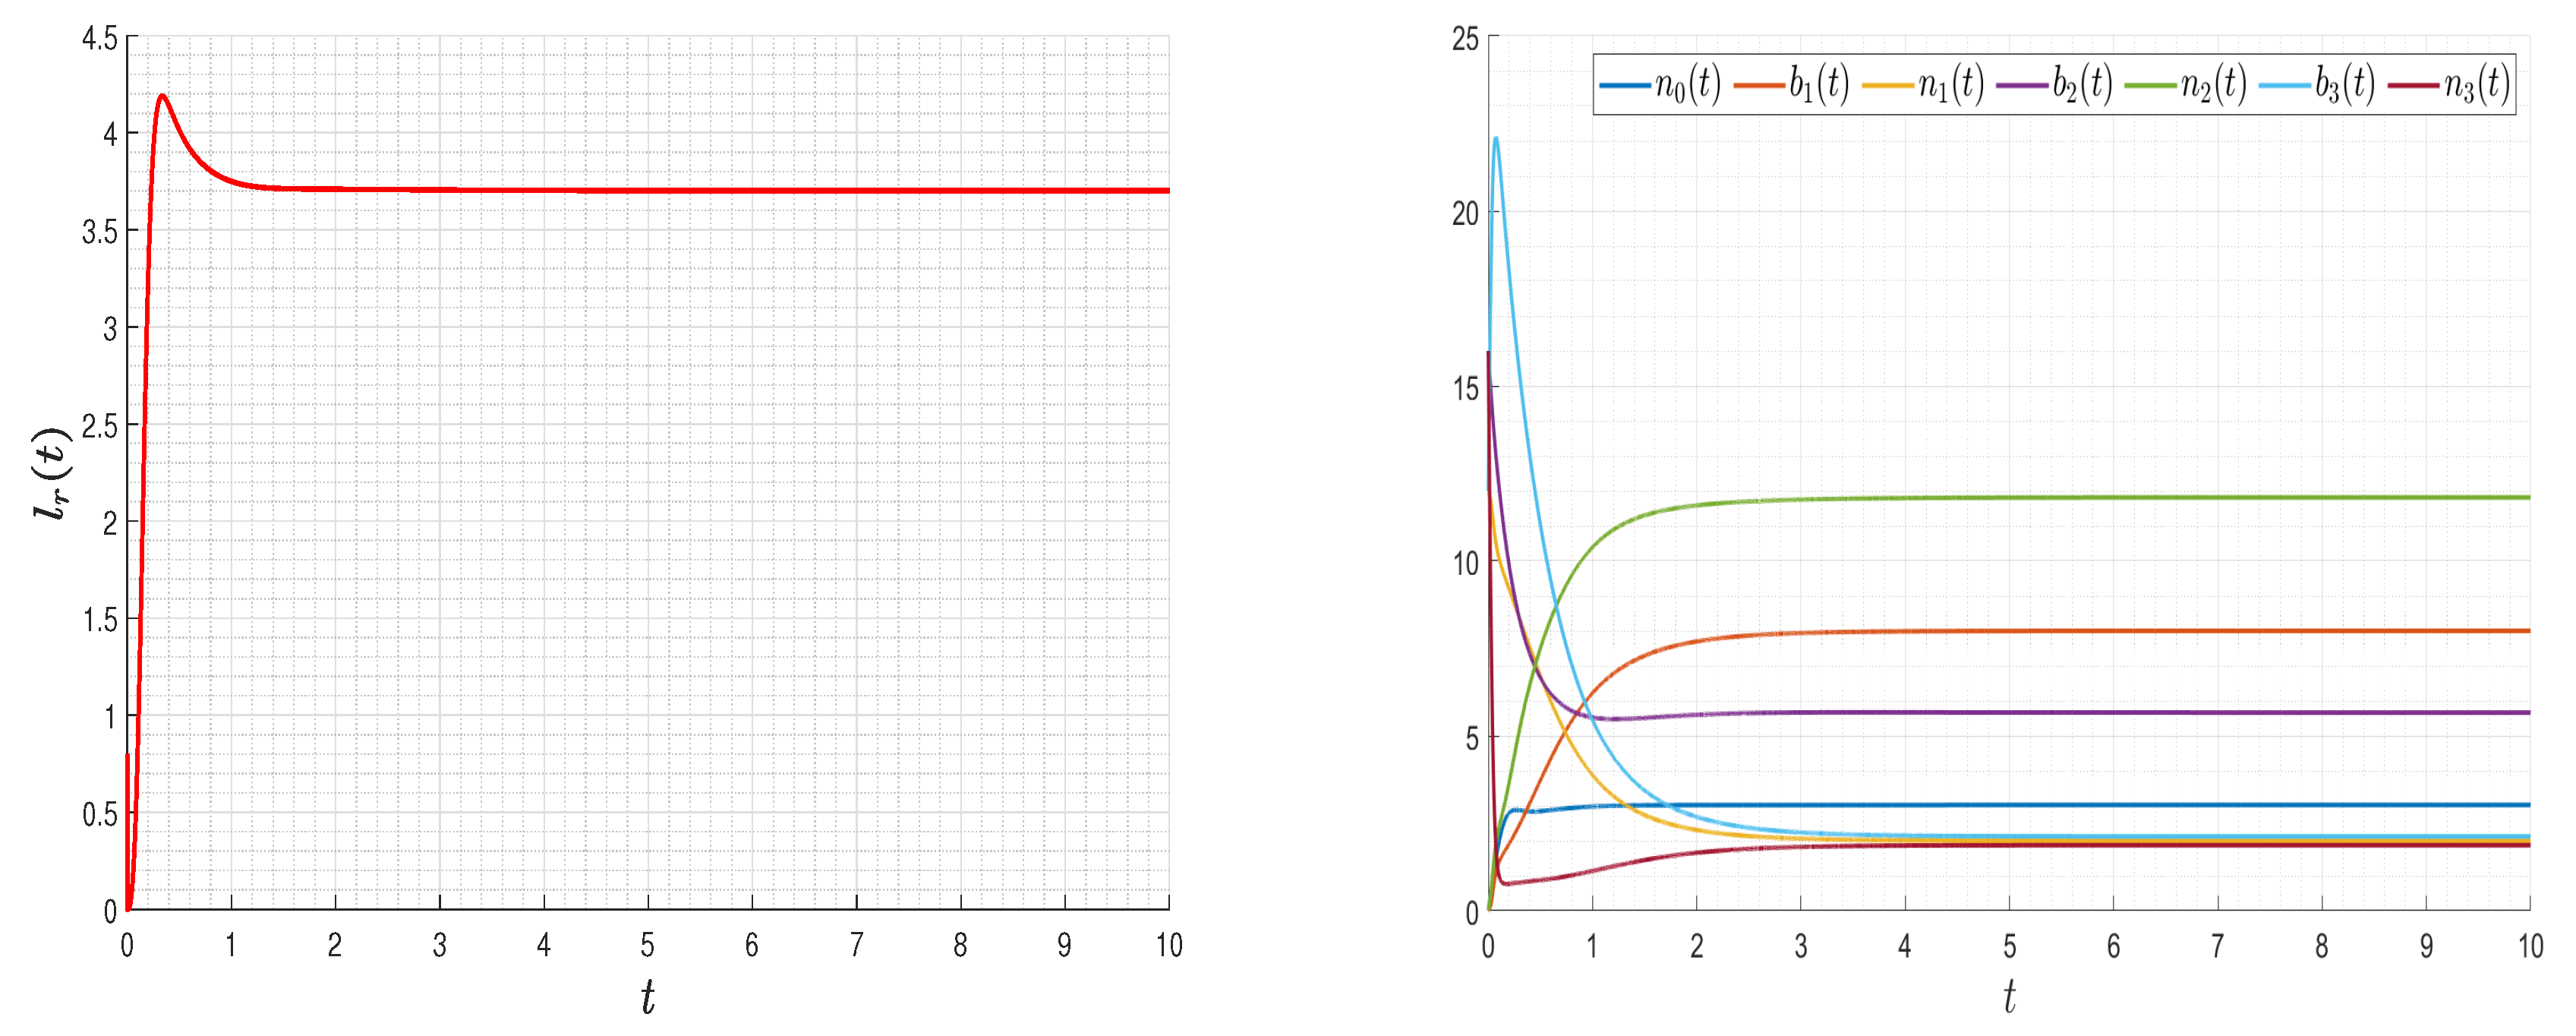
We suppose that the control, , in the following examples is a time-varying function, , an initial value of , and bounds are provided by and . With a final time of , we take into consideration an initial state of . Appendix A contains the used numerical scheme to approximate the control problem. The optimal solution is extremely smooth, as shown in Figure 12, Figure 13 and Figure 14. By increasing the -values, the -values fall; however, by increasing the -values, the -values increase. Note that varying the values of , , and does not significantly impact the end values for the biomass and organic matter. The optimal strategy approach makes it possible to optimize the control values (costs) and reduce the organic matter.
Figure 12.
The optimal strategy’s impact for , , .
Figure 13.
The optimal strategy’s impact for , , .
Figure 14.
The optimal strategy’s impact for , , .
8. Conclusions
This study presents a detailed mathematical model to analyze the dynamics of a three-tiered microbial food web in a chemostat under leachate recirculation. The model captures the complex interactions between chlorophenol degraders, phenol degraders, and methanogens, incorporating the inhibitory effects of hydrogen on microbial growth. Through rigorous qualitative analysis, we established the existence and stability conditions for various equilibrium states, demonstrating that the persistence of all three bacterial species is ensured under biologically reasonable assumptions.
The reduction of the seven-dimensional system to a three-dimensional one simplified the analysis while retaining essential biological insights. Analysis of the equilibria’s local and global stability is performed. This study concludes that the asymptotic persistence of the three bacteria is ensured given general assumptions of monotonicity on the growth rates. Furthermore, the introduction of an optimal control strategy for leachate recirculation provides a practical framework for minimizing organic matter accumulation while optimizing reactor performance. Numerical simulations validated the theoretical findings, illustrating the model’s applicability in predicting microbial dynamics under different conditions.
Future research could extend this work by incorporating experimental validation to confirm model predictions, exploring additional inhibitory factors, or refining the optimal control approach for industrial-scale applications. Such advancements would further bridge the gap between theoretical modeling and real-world bioreactor management, enhancing the efficiency of anaerobic digestion processes in waste treatment and biogas production.
In summary, this study contributes a robust theoretical foundation for understanding microbial interactions in engineered ecosystems and offers actionable insights for optimizing leachate recirculation strategies in bioreactors.
Author Contributions
Conceptualization, F.A.A.N., M.E.H. and B.S.A.; methodology, F.A.A.N., M.E.H. and B.S.A.; software, F.A.A.N., M.E.H. and B.S.A.; investigation, F.A.A.N., M.E.H. and B.S.A.; visualization, F.A.A.N., M.E.H. and B.S.A.; writing—original draft, F.A.A.N., M.E.H. and B.S.A.; writing—review and editing, F.A.A.N., M.E.H. and B.S.A. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by the Deanship of Scientific Research, Vice Presidency for Graduate Studies and Scientific Research, King Faisal University, Saudi Arabia [Grant No. KFU252345].
Data Availability Statement
The original contributions presented in the study are included in the article; further inquiries can be directed to the corresponding author.
Acknowledgments
The authors thank King Faisal University for its technical and financial support. The authors are also grateful to the anonymous reviewers for their many constructive suggestions, which helped to improve the presentation of the paper.
Conflicts of Interest
The authors declare no conflicts of interest.
Appendix A. Suitable Numerical Scheme
Let . Let , , , , , , , , , , , , , and approaching , , , , , , , , , , , , , and at . A first-order backward-difference scheme will be used for the adjoint variables estimation, and an improvement of the Gauss–Seidel-like implicit finite-difference scheme will be used for the state variables estimation.
Hence, will be calculated as follows: provided that and . Thus, we will use the Algorithm A1 given hereafter.
| Algorithm A1 Optimal leachate recirculation strategy procedure |
| , , , , , , , , , , , , , , , for to do end |
References
- Zhao, X.; Li, L.; Wu, D.; Xiao, T.; Ma, Y.; Peng, X. Modified Anaerobic Digestion Model No. 1 for modeling methane production from food waste in batch and semi-continuous anaerobic digestions. Bioresour. Technol. 2019, 271, 109–117. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Daoud, Y.; Abdellatif, N.; Sari, T.; Harmand, J. Steady state analysis of a syntrophic model: The effect of a new input substrate concentration. Math. Model. Nat. Phenom. 2018, 13, 31. [Google Scholar] [CrossRef] [Scilit]
- Fekih-Salem, R.; Daoud, Y.; Abdellatif, N.; Sari, T. A mathematical model of anaerobic digestion with syntrophic relationship, substrate inhibition and distinct removal rates. SIAM J. Appl. Dyn. Syst. 2020, 20, 1621–1654. [Google Scholar] [CrossRef] [Scilit]
- Sari, T.; Harmand, J. A model of a syntrophic relationship between two microbial species in a chemostat including maintenance. Math. Biosci. 2016, 275, 1–9. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Reinhart, D.R. A Review Of Recent Studies On The Sources Of Hazardous Compounds Emitted From Solid Waste Landfills: A U.S. Experience. Waste Manag. Res. 1993, 11, 257–268. [Google Scholar] [CrossRef] [Scilit]
- Paxéus, N. Organic compounds in municipal landfill leachates. Water Sci. Technol. 2000, 42, 323–333. [Google Scholar] [CrossRef] [Scilit]
- Lou, S.N.; Lin, Y.S.; Hsu, Y.S.; Chiu, E.M.; Ho, C.T. Soluble and insoluble phenolic compounds and antioxidant activity of immature calamondin affected by solvents and heat treatment. Food Chem. 2014, 161, 246–253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Batstone, D.; Keller, J.; Angelidaki, I.; Kalyuzhnyi, S.; Pavlostathis, S.; Rozzi, A.; Sanders, W.; Siegrist, H.; Vavilin, V. The IWA Anaerobic Digestion Model No 1 (ADM1). Water Sci. Technol. 2002, 45, 65–73. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- El Hajji, M. Influence of the presence of a pathogen and leachate recirculation on a bacterial competition. Int. J. Biomath. 2024. [Google Scholar] [CrossRef] [Scilit]
- Wade, M.J.; Pattinson, R.; Parker, N.; Dolfing, J. Emergent behaviour in a chlorophenol35 mineralising three-tiered microbial ‘food web’. J. Theor. Biol. 2016, 389, 171–186. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sari, T.; Wade, M. Generalised approach to modelling a three-tiered microbial food-web. Math. Biosci. 2017, 291, 21–37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Almuashi, H.H.; Almuallem, N.A.; El Hajji, M. The Effect of Leachate Recycling on the Dynamics of Two Competing Bacteria with an Obligate One-Way Beneficial Relationship in a Chemostat. Mathematics 2024, 12, 3819. [Google Scholar] [CrossRef] [Scilit]
- Almuallem, N.A.; El Hajji, M. How Can Viruses Affect the Growth of Zooplankton on Phytoplankton in a Chemostat? Mathematics 2025, 13, 1192. [Google Scholar] [CrossRef] [Scilit]
- El Hajji, M.; Chorfi, N.; Jleli, M. Mathematical modelling and analysis for a three-tiered microbial food web in a chemostat. Electron. J. Diff. Eqns. 2017, 2017, 1–13. [Google Scholar]
- Weedermann, M.; Seo, G.; Wolkowicz, G.S.K. Mathematical model of anaerobic digestion in a chemostat: Effects of syntrophy and inhibition. J. Biol. Dyn. 2013, 7, 59–85. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Smith, H.L.; Waltman, P. The Theory of the Chemostat. In Dynamics of Microbial Competition; Cambridge Studies in Mathematical Biology; Cambridge University Press: Cambridge, UK, 1995; Volume 13. [Google Scholar] [CrossRef] [Scilit]
- Teschl, G. Graduate Studies in Mathematics. InOrdinary Differential Equations and Dynamical Systems; American Mathematical Society: Washington, DC, USA, 2012; Volume 140. [Google Scholar]
- Thieme, H.R. Convergence results and a Poincaré-Bendixson trichotomy for asymptotically autonomous differential equations. J. Math. Biol. 1992, 30, 755–763. [Google Scholar] [CrossRef] [Scilit]
- Fleming, W.; Rishel, R. Deterministic and Stochastic Optimal Control; Springer: New York, NY, USA, 1975. [Google Scholar] [CrossRef] [Scilit]
- Lenhart, S.; Workman, J.T. Optimal Control Applied to Biological Models; Chapman and Hall: Boca Raton, FL, USA, 2007. [Google Scholar] [CrossRef] [Scilit]
- Pontryagin, L.S.; Boltyanskii, V.G.; Gamkrelidze, R.V.; Mishchenko, E.F.; Trirogoff, K.N.; Neustadt, L.W. The Mathematical Theory of Optimal Processes; CRC Press: Boca Raton, FL, USA, 1987. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).