
Uncovering the Genetic Basis of Grain Protein Content and Wet Gluten Content in Common Wheat (Triticum aestivum L.)


Abstract
1. Introduction
2. Results
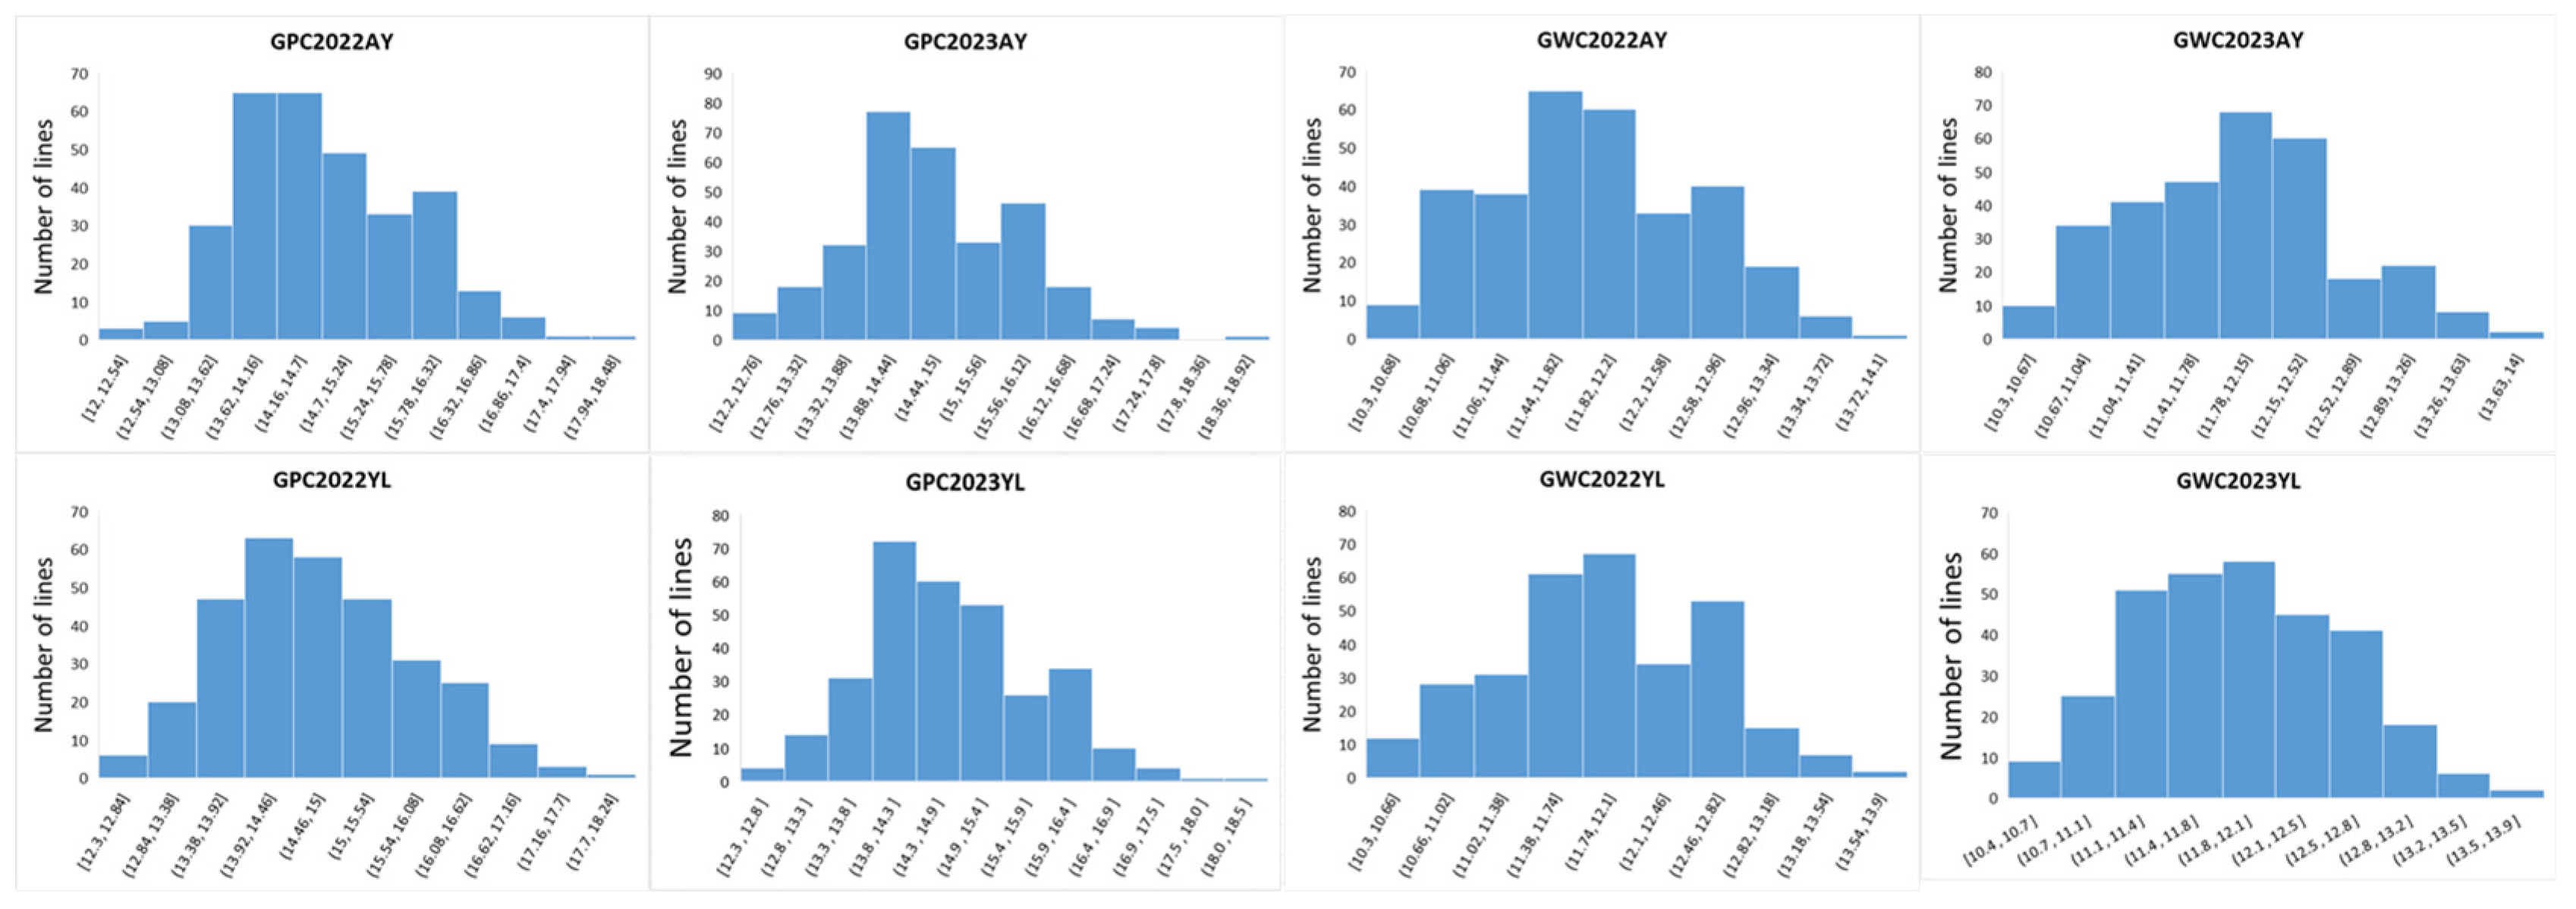
2.1. Phenotypic Evaluation
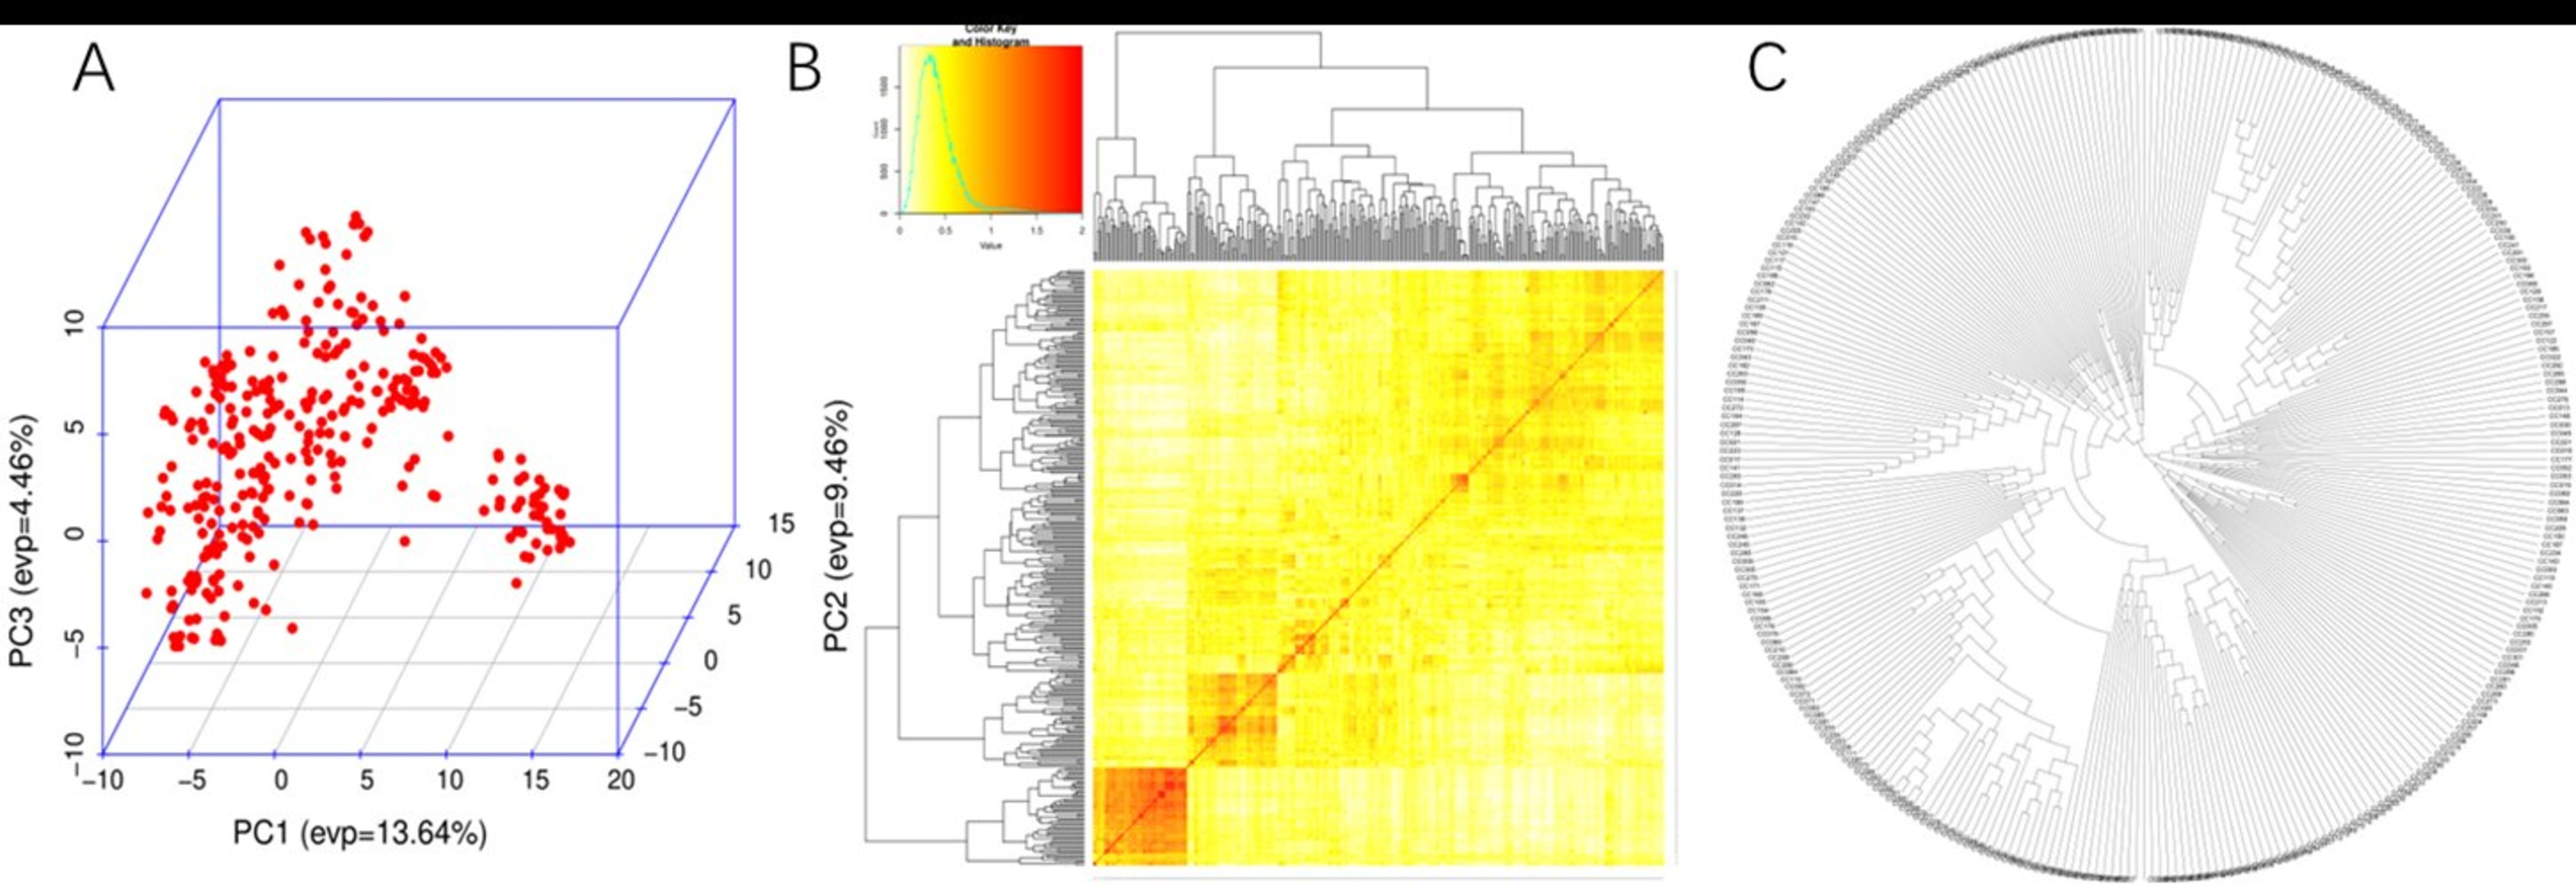
2.2. Genotyping and Population Structure Analysis
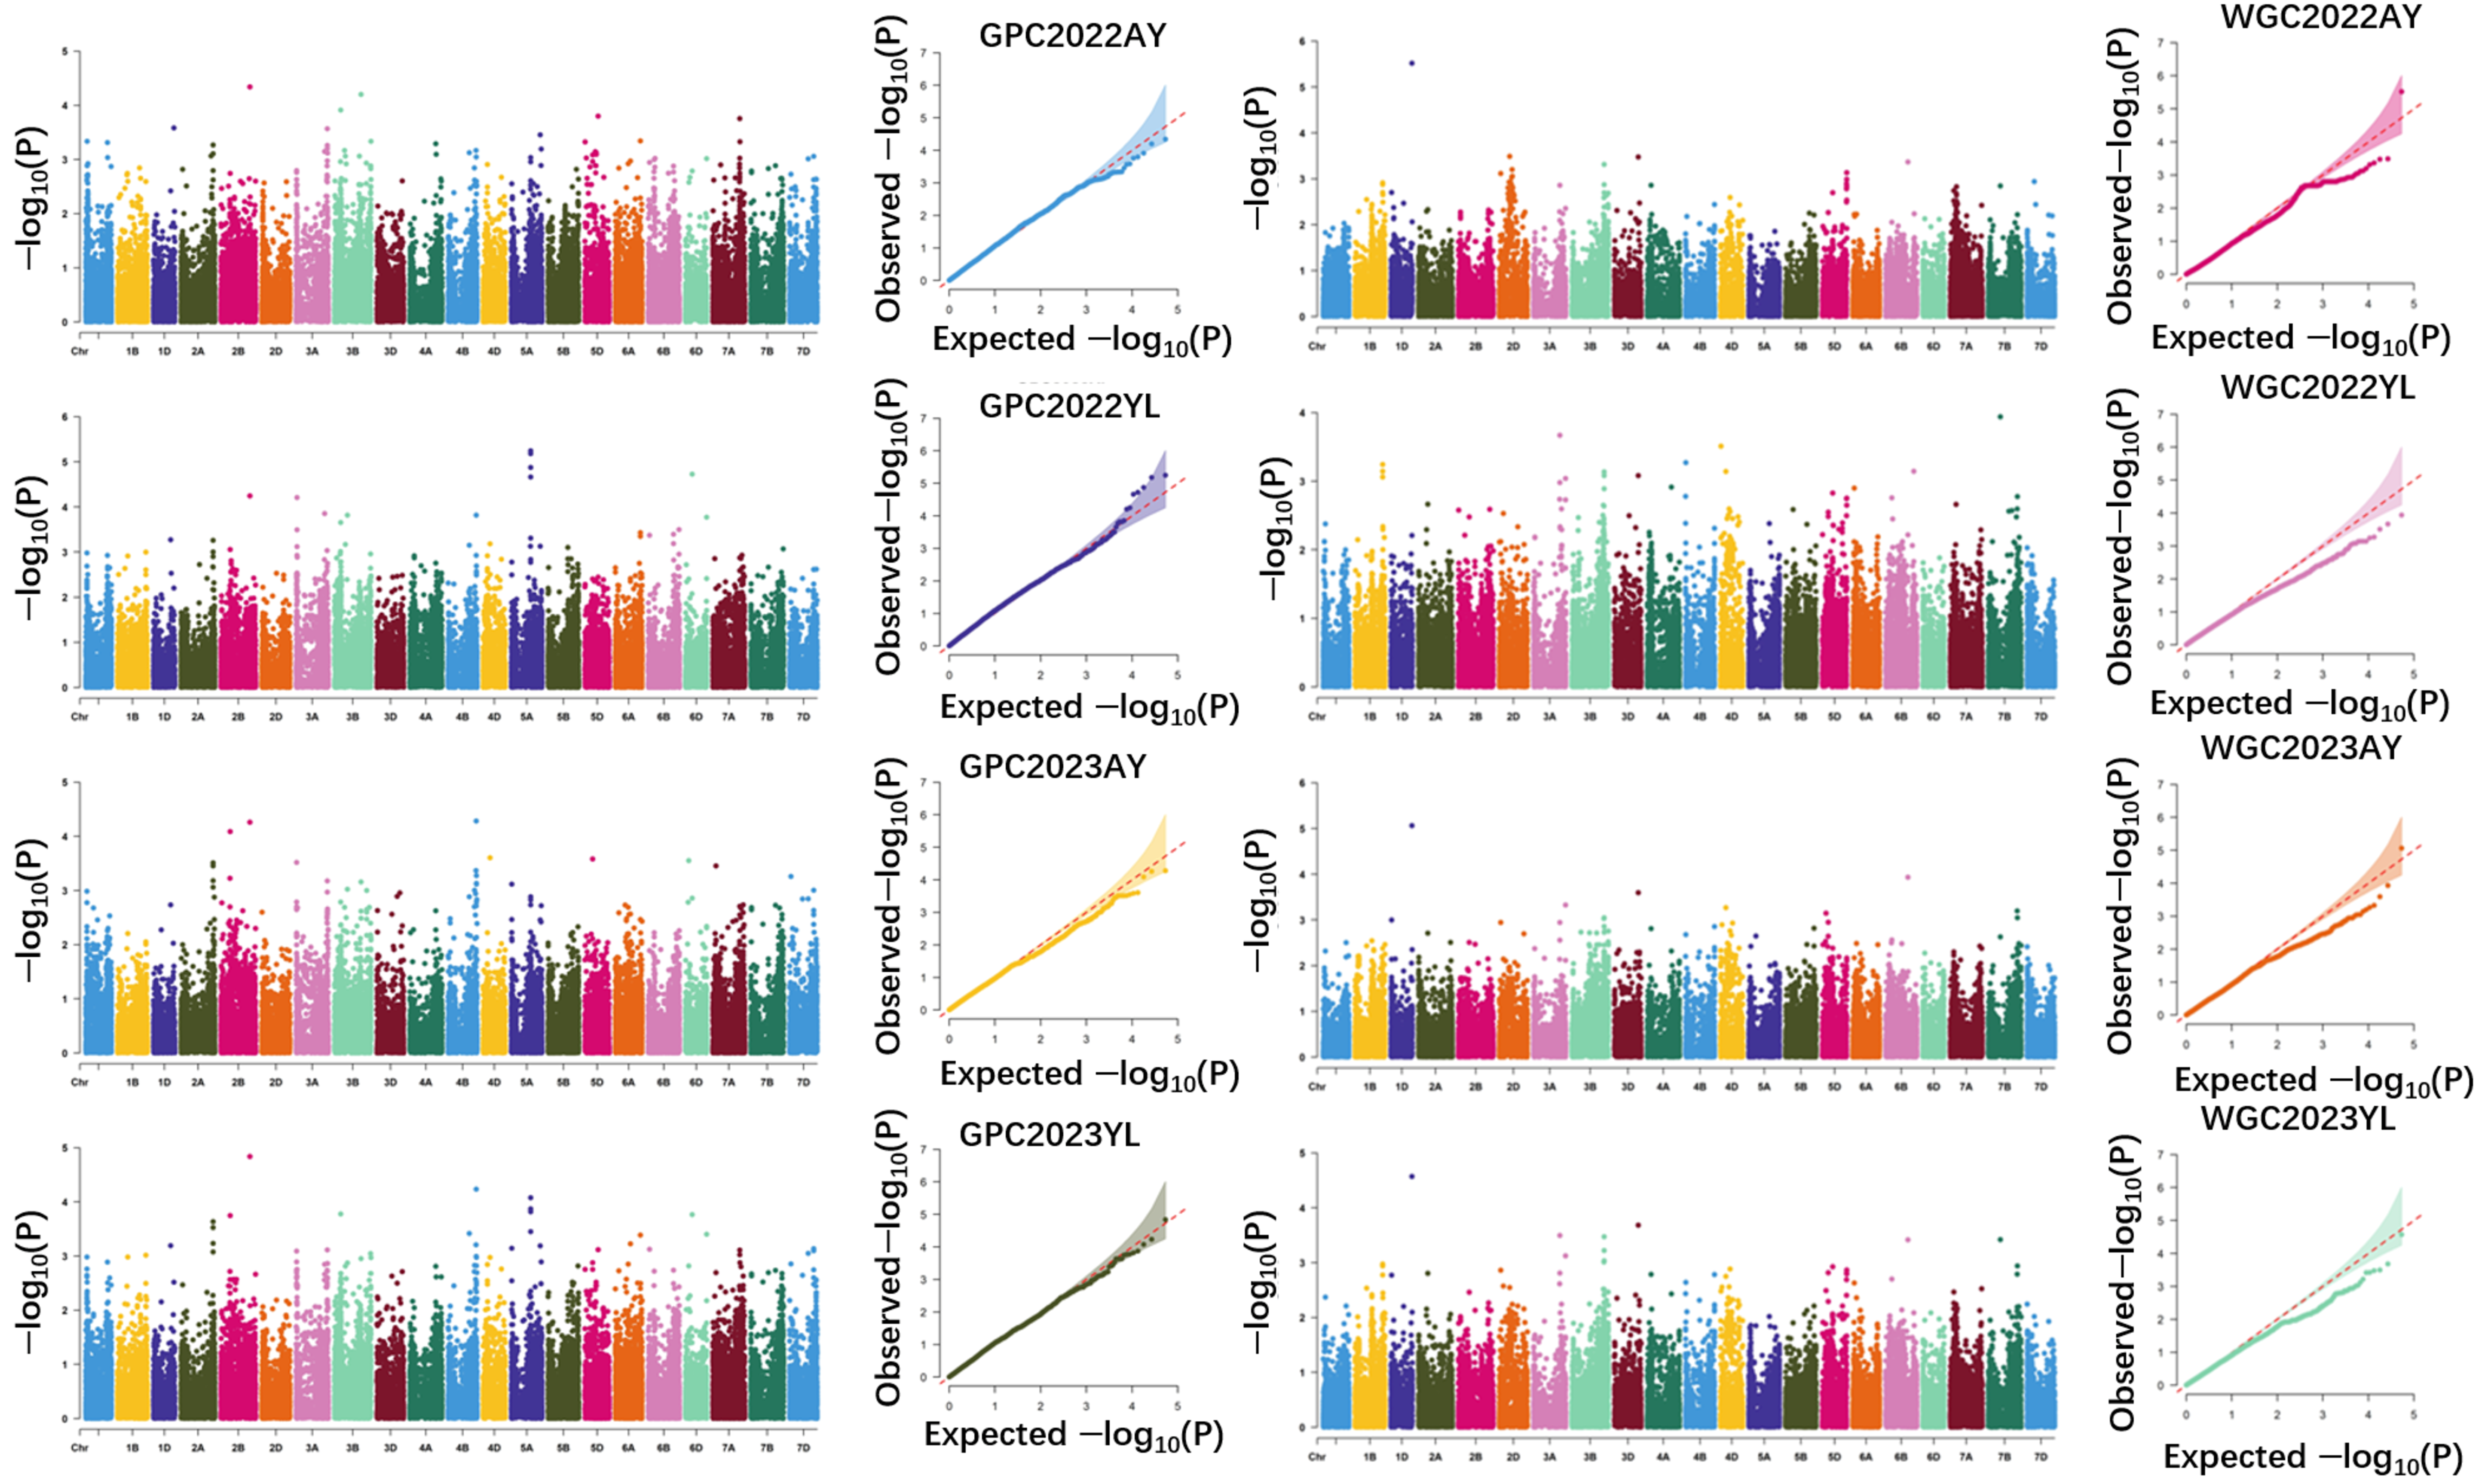
2.3. GWAS for Grain Protein Content and Wet Gluten Content
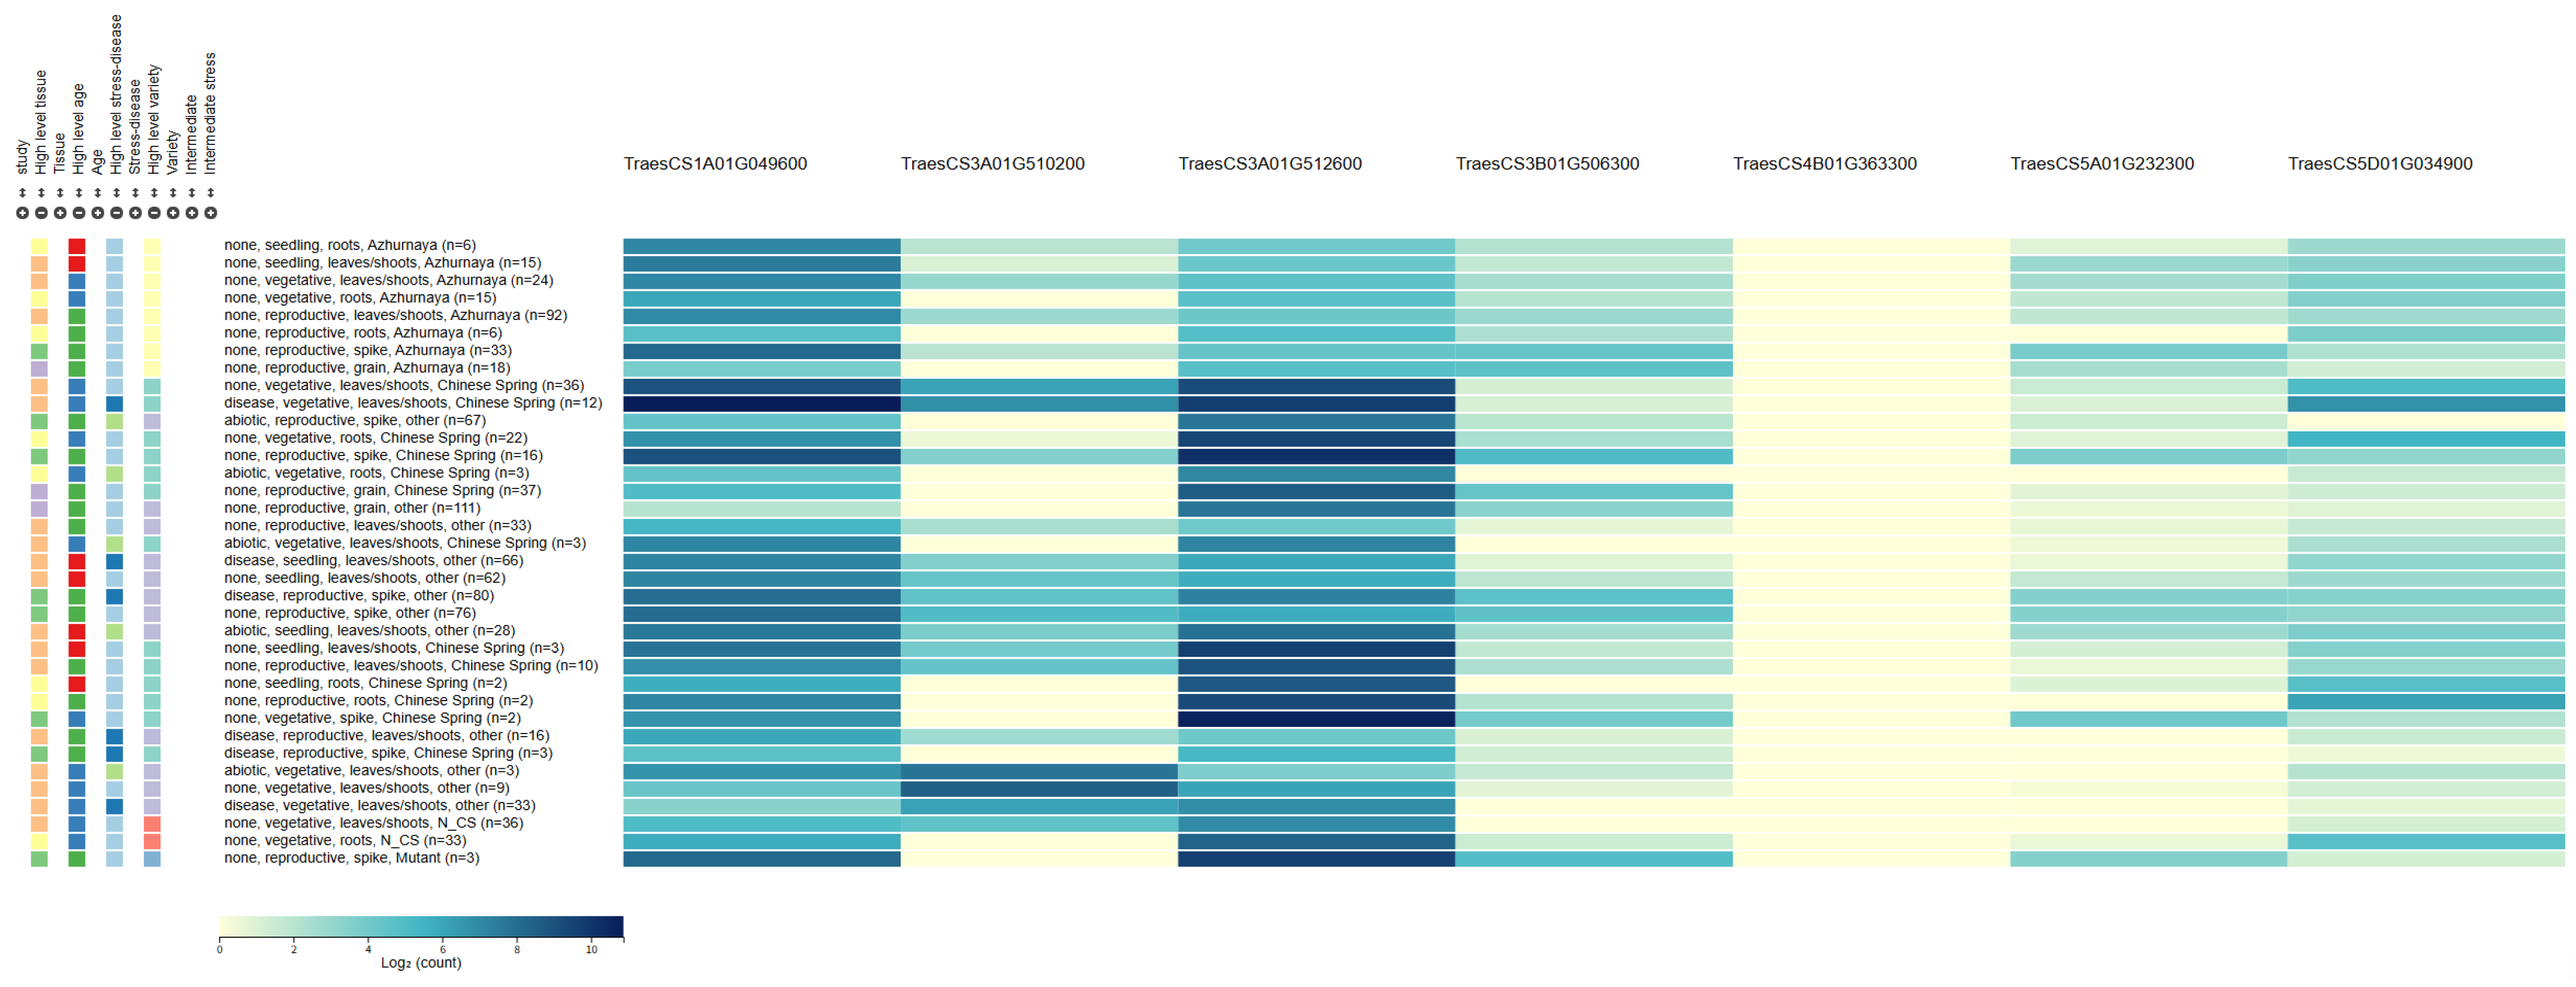
2.4. Candidate Gene Identification
2.5. Five Breeding Available KASP Markers Were Developed and Validation
3. Discussion
3.1. Loci for Grain Protein Content
3.2. Loci for Wet Gluten Content
3.3. The Candidate Genes for Grain Protein Content and Wet Gluten Content
3.4. The Validation of the KASP Markers for Grain Protein Content and Wet Gluten Content
4. Materials and Methods
4.1. Plant Materials and Field Trials
4.2. Genotyping and Population Structure Analysis
4.3. Phenotyping Analysis
4.4. Association Analysis and Candidate Gene Identification
4.5. KASP Marker Development and Validation
5. Conclusions
Author Contributions
Funding
Data Availability Statement
Conflicts of Interest
Abbreviations
| GWAS | Genome-wide association study |
| KASP | Kompetitive allele-specific PCR |
| GPC G | Rain protein content |
| WGC | Wet gluten content |
| QTL | Quantitative trait loci |
| SNP | Single nucleotide polymorphism |
Appendix A

| Name | Subgroup | Grain Protein Content (%) | Wet Gluten Content (%) | ||||||
|---|---|---|---|---|---|---|---|---|---|
| E1 | E2 | E3 | E4 | E1 | E2 | E3 | E4 | ||
| 04Zhong36 | 3 | 15.1 | 15.8 | 14.7 | 15.2 | 11.9 | 11.1 | 11.2 | 11.4 |
| 19CA27 | 1 | 15.9 | 14.7 | 15.8 | 15.5 | 12.2 | 11.8 | 12.3 | 12.1 |
| 19CA97 | 1 | 15.8 | 16.2 | 16.2 | 16.1 | 12.3 | 12.8 | 12.5 | 12.5 |
| Anke1702 | 2 | 13.8 | 14 | 14.5 | 14.1 | 10.9 | 11 | 11.3 | 11.1 |
| Anke1704 | 2 | 15.5 | 15.3 | 14.9 | 15.2 | 12.8 | 12.6 | 12.5 | 12.6 |
| Anke1901 | 2 | 13.8 | 13.8 | 14.2 | 13.9 | 12.1 | 11.9 | 12.1 | 12.0 |
| Anke1908 | 2 | 12.2 | 12.6 | 12.3 | 12.4 | 11.5 | 11.7 | 11.6 | 11.6 |
| Anke2006 | 2 | 13.9 | 14.1 | 14.4 | 14.1 | 13.8 | 12.7 | 13 | 13.2 |
| Anke2007 | 2 | 14.3 | 13.3 | 13.1 | 13.6 | 12.8 | 12.3 | 12.7 | 12.6 |
| Anke2008 | 2 | 14.3 | 14.3 | 14.6 | 14.4 | 12.8 | 12.2 | 12.6 | 12.5 |
| Anke203 | 1 | 13.5 | 12.8 | 12.8 | 13.0 | 11.4 | 11.1 | 11.4 | 11.3 |
| Anong1589 | - | 14.2 | 14 | 13.5 | 13.9 | 13.1 | 13.3 | 12.8 | 13.1 |
| Anong1928 | - | 15 | 14.5 | 14.8 | 14.8 | 11.7 | 12 | 12.4 | 12.0 |
| Bainong207 | 1 | 12.8 | 14 | 13.7 | 13.5 | 11.5 | 11.7 | 12.1 | 11.8 |
| BainongChengzhu21 | 3 | 13.5 | 14.2 | 14 | 13.9 | 12 | 11.9 | 12 | 12.0 |
| Baofeng1903 | 3 | 13.1 | 12.6 | 13.7 | 13.1 | 11.2 | 10.8 | 11.5 | 11.2 |
| Baofeng216 | 2 | 14.3 | 14 | 13.6 | 14.0 | 13.5 | 13.1 | 12.7 | 13.1 |
| Baoliang5hao | 1 | 15.3 | 14.9 | 15.1 | 15.1 | 12 | 11.9 | 12 | 12.0 |
| Changmai20 | 1 | 13.8 | 13.5 | 14.4 | 13.9 | 11.1 | 10.8 | 11.3 | 11.1 |
| Cunmai16hao | 3 | 16.4 | 15.8 | 16.8 | 16.3 | 11.7 | 11.7 | 12.2 | 11.9 |
| Cunmai35 | 2 | 14.1 | 14.5 | 14.4 | 14.3 | 12.7 | 12.7 | 12.9 | 12.8 |
| Dehongfumai21 | 3 | 15 | 15.8 | 15.6 | 15.5 | 11.7 | 12.1 | 11.3 | 11.7 |
| Fanmai26 | 2 | 14.2 | 14.7 | 14.1 | 14.3 | 13.2 | 13.5 | 13.4 | 13.4 |
| Fanyuemai32 | - | 14.4 | 14.2 | 13.9 | 14.2 | 12.2 | 12.2 | 11.5 | 12.0 |
| FengdeCunmai16hao | 1 | 15.5 | 15 | 14.8 | 15.1 | 12.1 | 12.2 | 12.4 | 12.2 |
| Fuma916 | - | 15.6 | 14.9 | 15.9 | 15.5 | 12.8 | 12.9 | 12.9 | 12.9 |
| Fumai16 | 2 | 14.5 | 14.8 | 14.1 | 14.5 | 10.9 | 11.5 | 11 | 11.1 |
| Fumai33 | 1 | 14.9 | 14.2 | 13.3 | 14.1 | 11.8 | 12 | 12 | 11.9 |
| Guanmai13 | 3 | 14.2 | 14.3 | 13.6 | 14.0 | 11.2 | 11.1 | 10.9 | 11.1 |
| Hengmai175345 | 1 | 14.1 | 14.5 | 14.3 | 14.3 | 12 | 12 | 12.3 | 12.1 |
| Hengmai175364 | 2 | 13.8 | 14.1 | 13.9 | 13.9 | 11 | 11.6 | 11.4 | 11.3 |
| Huacheng138 | 2 | 14.3 | 14.8 | 15 | 14.7 | 12 | 12.4 | 12.1 | 12.2 |
| Huacheng865 | 2 | 13.9 | 13.5 | 14.1 | 13.8 | 12.4 | 11.9 | 12.3 | 12.2 |
| Huacheng9137 | 2 | 16.5 | 16.2 | 16.5 | 16.4 | 11 | 10.9 | 10.9 | 10.9 |
| Huacheng916 | 2 | 16.1 | 14.6 | 15.1 | 15.3 | 12.3 | 11.6 | 11.7 | 11.9 |
| Huaimai2118 | 3 | 14.7 | 14.3 | 14.4 | 14.5 | 13 | 13.2 | 12.9 | 13.0 |
| Huaimai40 | 2 | 14 | 13.7 | 14.5 | 14.1 | 11.2 | 10.9 | 11.2 | 11.1 |
| Huaimai404 | 3 | 15.6 | 16.3 | 16.4 | 16.1 | 11.7 | 11.5 | 11.9 | 11.7 |
| Huaiming36 | - | 14.8 | 14.8 | 14.7 | 14.8 | 12.9 | 12.4 | 12 | 12.4 |
| Huake20212 | - | 15.3 | 15 | 14.2 | 14.8 | 12.6 | 12.2 | 12.6 | 12.5 |
| Huamai17v65 | 2 | 13.4 | 13.9 | 13.7 | 13.7 | 11.6 | 11.7 | 11.1 | 11.5 |
| Huamai2003 | 1 | 13.8 | 14.5 | 13.9 | 14.1 | 10.6 | 11.2 | 10.8 | 10.9 |
| Huamai2100 | 2 | 14.6 | 14.3 | 14.9 | 14.6 | 11.2 | 11.7 | 11.7 | 11.5 |
| Jiamai208 | 1 | 14.9 | 14.8 | 14.3 | 14.7 | 10.6 | 10.9 | 10.4 | 10.6 |
| Jimai196 | 2 | 16.3 | 16 | 16.1 | 16.1 | 12.2 | 11.9 | 12.3 | 12.1 |
| Jimai20 | 2 | 16.1 | 15.9 | 16 | 16.0 | 10.6 | 10.6 | 11.3 | 10.8 |
| Jimai211 | 1 | 15.2 | 15.6 | 15 | 15.3 | 12.1 | 11.9 | 12.3 | 12.1 |
| Jimai418 | 2 | 14 | 14.5 | 13.8 | 14.1 | 12.3 | 11.2 | 11.9 | 11.8 |
| Jìmài44 | - | 15.5 | 15 | 15.5 | 15.3 | 11.9 | 11.7 | 11.8 | 11.8 |
| Jinhedao17278 | - | 13 | 13.4 | 13.5 | 13.3 | 11.1 | 10.8 | 11.4 | 11.1 |
| Jiushenghe169 | 2 | 15.1 | 13.9 | 14.6 | 14.5 | 11 | 11.1 | 11.2 | 11.1 |
| Jiyuanmai20 | - | 14 | 14.6 | 14 | 14.2 | 11.7 | 11.7 | 11.5 | 11.6 |
| Kedaxia1026 | - | 14.9 | 14.4 | 14.4 | 14.6 | 11.3 | 10.7 | 10.8 | 10.9 |
| Kedaxia116 | - | 14.6 | 14.7 | 14.1 | 14.5 | 11.8 | 11.8 | 11.8 | 11.8 |
| Liangke6hao | 2 | 14 | 13.9 | 13.6 | 13.8 | 13.1 | 12.6 | 13.1 | 12.9 |
| Lianmai1901 | 2 | 15.4 | 14.8 | 14.2 | 14.8 | 12.1 | 11.7 | 12.4 | 12.1 |
| Liuxia526 | - | 15 | 14 | 14.2 | 14.4 | 12.3 | 11.9 | 11.9 | 12.0 |
| Longmai1hao | 2 | 13.6 | 12.6 | 13.2 | 13.1 | 10.8 | 10.6 | 11.5 | 11.0 |
| Lunxuan136 | 3 | 15.1 | 15.9 | 14.7 | 15.2 | 11.7 | 11.9 | 11.5 | 11.7 |
| Lunxuan148 | 2 | 15.9 | 16.3 | 16.5 | 16.2 | 12.1 | 12.3 | 12.5 | 12.3 |
| Lunxuan369 | 1 | 14.6 | 14.1 | 14.4 | 14.4 | 11.4 | 11.2 | 11.6 | 11.4 |
| Luomai26 | 3 | 14.9 | 15.3 | 15.3 | 15.2 | 11.5 | 10.8 | 10.9 | 11.1 |
| Luomai28 | 2 | 16.1 | 15.6 | 15.4 | 15.7 | 11.1 | 11.8 | 11.7 | 11.5 |
| Luomai44 | 1 | 13.8 | 13.7 | 14.2 | 13.9 | 11 | 10.9 | 11.4 | 11.1 |
| Luomai45 | 1 | 14.1 | 14.8 | 13.6 | 14.2 | 11 | 11.3 | 10.9 | 11.1 |
| Luomai49 | 1 | 16.7 | 16.4 | 16.1 | 16.4 | 11.3 | 11 | 10.3 | 10.9 |
| Luomai50 | 1 | 13.9 | 15.1 | 15.2 | 14.7 | 11 | 11.3 | 10.9 | 11.1 |
| Luomai54 | 1 | 16.4 | 16.1 | 16.1 | 16.2 | 10.8 | 10.8 | 11.3 | 11.0 |
| Luomai56 | 2 | 15.1 | 14.2 | 15.2 | 14.8 | 12.1 | 11.8 | 11.6 | 11.8 |
| Luomai59 | 1 | 13.5 | 13.1 | 14.9 | 13.8 | 11.5 | 11.3 | 11.4 | 11.4 |
| Luoqing1905 | - | 15.3 | 15.4 | 15.6 | 15.4 | 12.5 | 12 | 12.4 | 12.3 |
| Luoqingfeng2101 | - | 13.7 | 14.5 | 13.9 | 14.0 | 10.7 | 11.1 | 10.6 | 10.8 |
| Luoqingfeng7011 | - | 13.4 | 13.6 | 13.9 | 13.6 | 10.8 | 10.7 | 10.7 | 10.7 |
| Luoqingmai109 | - | 13.5 | 13.4 | 13.6 | 13.5 | 11.6 | 11.8 | 11.6 | 11.7 |
| Luoqingmai40 | - | 16.4 | 15.5 | 15.7 | 15.9 | 11.6 | 11.2 | 10.9 | 11.2 |
| Luoqingmai56 | - | 12.6 | 13.2 | 13.2 | 13.0 | 11.5 | 11.9 | 12.1 | 11.8 |
| Luoqingmai69 | - | 14.2 | 13.9 | 13.9 | 14.0 | 13.4 | 13.1 | 13.2 | 13.2 |
| Luoqingmai70 | - | 15.7 | 14.3 | 14.4 | 14.8 | 10.7 | 10.6 | 10.5 | 10.6 |
| Nongda759 | 2 | 14 | 14 | 14.2 | 14.1 | 12.5 | 12.5 | 12.7 | 12.6 |
| Nongke1132 | 2 | 16.3 | 15.9 | 15.4 | 15.9 | 12.2 | 12.5 | 12.5 | 12.4 |
| Nongxin699 | 2 | 15.8 | 15.7 | 15.7 | 15.7 | 11.9 | 11.6 | 11.7 | 11.7 |
| Pingan0518 | - | 15.7 | 16 | 15 | 15.6 | 11.7 | 11.9 | 11.7 | 11.8 |
| Pingan18 | - | 15.6 | 14.9 | 15.4 | 15.3 | 12.8 | 12.8 | 12.5 | 12.7 |
| Puling300 | - | 13.6 | 13.9 | 14.1 | 13.9 | 11.1 | 11.6 | 11.4 | 11.4 |
| Puling35038 | - | 13.8 | 13.7 | 14.2 | 13.9 | 10.8 | 10.3 | 10.5 | 10.5 |
| Pumai126 | 1 | 15.2 | 15 | 15.9 | 15.4 | 11.6 | 12 | 11.6 | 11.7 |
| Pumai127 | 1 | 14.1 | 13.5 | 13.3 | 13.6 | 11 | 12.1 | 11.6 | 11.6 |
| Pumai157 | 1 | 15.8 | 15 | 15 | 15.3 | 12.3 | 12.4 | 12 | 12.2 |
| Pumai186 | 1 | 14.5 | 15 | 15.6 | 15.0 | 11.9 | 11.6 | 11.8 | 11.8 |
| Puxing26hao | 3 | 15.5 | 15.4 | 15.7 | 15.5 | 11.5 | 11 | 11.5 | 11.3 |
| Puxing35hao | 1 | 15.3 | 15.1 | 15.5 | 15.3 | 10.8 | 11 | 10.8 | 10.9 |
| Ruihua519 | 2 | 17 | 17.7 | 18.1 | 17.6 | 13.1 | 12.9 | 12.3 | 12.8 |
| Ruihuamai236 | 3 | 14.2 | 13.5 | 13.8 | 13.8 | 12.9 | 13 | 12.7 | 12.9 |
| Ruihuamai513 | 1 | 17.6 | 17.1 | 15.2 | 16.6 | 11.6 | 11.1 | 11.4 | 11.4 |
| Saidemai216 | 1 | 13.3 | 13 | 12.6 | 13.0 | 12.2 | 11.5 | 11.7 | 11.8 |
| Saidemai5hao | 1 | 15.9 | 16.3 | 16 | 16.1 | 11.9 | 11.9 | 11.5 | 11.8 |
| Sanfengmai616 | 3 | 15.4 | 15.2 | 14.8 | 15.1 | 11.4 | 11.4 | 11.3 | 11.4 |
| Shangmai187 | 2 | 13.7 | 13.7 | 13.2 | 13.5 | 12.3 | 12.8 | 12.1 | 12.4 |
| Shangmai198 | 3 | 13 | 13.5 | 13.1 | 13.2 | 12.6 | 12.8 | 12.5 | 12.6 |
| Shangmai206 | 1 | 15.9 | 16 | 15.8 | 15.9 | 11.2 | 11.4 | 11.4 | 11.3 |
| Shanhe1029 | 2 | 14.8 | 15.2 | 14.9 | 15.0 | 12.9 | 13 | 13.4 | 13.1 |
| Shengmaiyuan789 | 1 | 14.1 | 14.9 | 13.7 | 14.2 | 11.6 | 11.3 | 10.6 | 11.2 |
| Shi15-6375 | 2 | 14.1 | 13.7 | 13.8 | 13.9 | 13.2 | 12.8 | 12.3 | 12.8 |
| Shunmai10hao | 1 | 14.4 | 15.6 | 15.5 | 15.2 | 11 | 11.4 | 11.3 | 11.2 |
| Taiheimai10hao | - | 15.6 | 14.1 | 15.1 | 14.9 | 12.3 | 12.6 | 12.5 | 12.5 |
| Tianmai116 | 1 | 15.7 | 15.9 | 15.2 | 15.6 | 10.8 | 11.1 | 10.5 | 10.8 |
| Tianmai159 | 1 | 14.9 | 14.6 | 14.8 | 14.8 | 12 | 12.1 | 12.2 | 12.1 |
| Tianmai160 | 1 | 14 | 14.2 | 14 | 14.1 | 12.9 | 12.8 | 12.6 | 12.8 |
| Tianmai177 | 1 | 15.2 | 15.5 | 15 | 15.2 | 11.6 | 11.7 | 11.6 | 11.6 |
| Tianmai196 | 1 | 14.1 | 14.2 | 14 | 14.1 | 11.6 | 11.5 | 10.8 | 11.3 |
| Tianmin360 | 3 | 16.6 | 15.9 | 16.8 | 16.4 | 11.2 | 11.4 | 11.7 | 11.4 |
| Tianning138 | 3 | 14.6 | 14.9 | 15.1 | 14.9 | 12.7 | 12.9 | 12.4 | 12.7 |
| Tianyikemai15 | 2 | 15.4 | 14.6 | 14.8 | 14.9 | 12.9 | 12.5 | 12.6 | 12.7 |
| Tuomai303 | - | 13.8 | 13.2 | 13.7 | 13.6 | 11.5 | 11.2 | 11.1 | 11.3 |
| Tuomai44 | - | 14.4 | 14.2 | 14.7 | 14.4 | 11.7 | 11.4 | 11.8 | 11.6 |
| Tuomai606 | - | 14.1 | 14.8 | 14.7 | 14.5 | 11.9 | 12.4 | 11.7 | 12.0 |
| Tuyu16 | - | 13.5 | 13 | 12.8 | 13.1 | 11.2 | 11.6 | 10.8 | 11.2 |
| W1 | 4 | 14.2 | 14.2 | 15.1 | 14.5 | 13 | 12.5 | 12.9 | 12.8 |
| W10 | 4 | 13.4 | 13.8 | 14.1 | 13.8 | 13.1 | 12.3 | 12.8 | 12.7 |
| W11 | 4 | 15.1 | 15.3 | 15.1 | 15.2 | 12.3 | 12.7 | 12.4 | 12.5 |
| W12 | 4 | 15.2 | 14.9 | 14.9 | 15.0 | 12 | 12.2 | 12.1 | 12.1 |
| W13 | 4 | 15 | 15.5 | 14.2 | 14.9 | 12.5 | 13.2 | 12 | 12.6 |
| W14 | 4 | 13.7 | 13.7 | 14.1 | 13.8 | 11.7 | 12.1 | 12.2 | 12.0 |
| W15 | 4 | 14.1 | 14.4 | 14 | 14.2 | 10.9 | 11.1 | 10.7 | 10.9 |
| W16 | 4 | 14.4 | 13.1 | 13.9 | 13.8 | 12.3 | 12.3 | 11.9 | 12.2 |
| W17 | 4 | 14.3 | 14 | 13.5 | 13.9 | 12 | 11.8 | 11.3 | 11.7 |
| W18 | 4 | 14.8 | 14 | 14.5 | 14.4 | 11.7 | 11.8 | 11.8 | 11.8 |
| W19 | 4 | 16.8 | 17 | 16.8 | 16.9 | 11.6 | 11.9 | 12.3 | 11.9 |
| W2 | 4 | 14.9 | 15 | 14.9 | 14.9 | 12 | 11.7 | 11.9 | 11.9 |
| W20 | 4 | 14.1 | 13.8 | 13.8 | 13.9 | 12 | 12.3 | 12.6 | 12.3 |
| W21 | 4 | 13.2 | 13.6 | 13.2 | 13.3 | 12.6 | 12.5 | 12.3 | 12.5 |
| W22 | 4 | 13.5 | 13.9 | 13.4 | 13.6 | 13.3 | 13.1 | 12.7 | 13.0 |
| W23 | 4 | 15.8 | 15.9 | 14.9 | 15.5 | 12.8 | 13.2 | 12.8 | 12.9 |
| W24 | 4 | 12 | 12.2 | 12.6 | 12.3 | 12.6 | 12.2 | 12.6 | 12.5 |
| W25 | 1 | 14.2 | 14.1 | 14.5 | 14.3 | 10.9 | 11.2 | 11.1 | 11.1 |
| W26 | 4 | 13.7 | 13.4 | 13 | 13.4 | 11.4 | 10.9 | 10.9 | 11.1 |
| W27 | 4 | 14 | 15.3 | 14.5 | 14.6 | 11.9 | 12 | 11.6 | 11.8 |
| W29 | 4 | 14.9 | 15.7 | 15.4 | 15.3 | 10.8 | 10.8 | 11.2 | 10.9 |
| W3 | 4 | 13.4 | 13.6 | 13.5 | 13.5 | 12.2 | 12.3 | 12 | 12.2 |
| W30 | 4 | 14.4 | 14.9 | 14.6 | 14.6 | 11.3 | 11.8 | 11.9 | 11.7 |
| W31 | 4 | 14.9 | 14.4 | 14.6 | 14.6 | 11.3 | 11.4 | 11.5 | 11.4 |
| W32 | 4 | 15.4 | 15.9 | 16.5 | 15.9 | 13.1 | 12.7 | 12.4 | 12.7 |
| W33 | 4 | 15.6 | 15.6 | 15.4 | 15.5 | 12.2 | 12.4 | 11.9 | 12.2 |
| W34 | 4 | 15.5 | 14.6 | 15.6 | 15.2 | 12.8 | 12.4 | 12.7 | 12.6 |
| W35 | 4 | 16.1 | 15.3 | 15.9 | 15.8 | 13.3 | 13.3 | 13.2 | 13.3 |
| W36 | 4 | 16.1 | 17.1 | 16.6 | 16.6 | 13.1 | 13.5 | 13.3 | 13.3 |
| W37 | 4 | 14 | 13.8 | 14.1 | 14.0 | 12 | 12.3 | 11.8 | 12.0 |
| W38 | 4 | 14.4 | 13.4 | 13.5 | 13.8 | 13.4 | 13.1 | 12.9 | 13.1 |
| W39 | 4 | 14.7 | 15.9 | 13.9 | 14.8 | 12.6 | 13.1 | 12.6 | 12.8 |
| W4 | 4 | 14 | 14.8 | 14.7 | 14.5 | 12.6 | 13.1 | 12.5 | 12.7 |
| W40 | 4 | 14.8 | 14.1 | 14.4 | 14.4 | 11.7 | 11.9 | 11.3 | 11.6 |
| W41 | 4 | 13.9 | 14.1 | 14 | 14.0 | 12.6 | 12.5 | 12.8 | 12.6 |
| W43 | 4 | 13.8 | 13.7 | 14.6 | 14.0 | 12.1 | 11.8 | 12.3 | 12.1 |
| W45 | 4 | 14.4 | 14.2 | 14.7 | 14.4 | 10.9 | 11 | 11.3 | 11.1 |
| W47 | 4 | 16.7 | 16 | 15.1 | 15.9 | 12.4 | 12.1 | 12 | 12.2 |
| W49 | 4 | 14.3 | 15 | 14.4 | 14.6 | 12 | 12.2 | 12 | 12.1 |
| W5 | 4 | 14 | 13.2 | 13.1 | 13.4 | 11.7 | 11.6 | 11.9 | 11.7 |
| W50 | 2 | 16.3 | 16 | 15.3 | 15.9 | 12.5 | 12.3 | 12.4 | 12.4 |
| W51 | 4 | 13.4 | 13.7 | 13.3 | 13.5 | 12.3 | 11.8 | 11.7 | 11.9 |
| W52 | 4 | 14 | 13.5 | 14.3 | 13.9 | 13.3 | 13 | 12.9 | 13.1 |
| W53 | 4 | 14.8 | 13.8 | 13.7 | 14.1 | 12.1 | 11.6 | 11.8 | 11.8 |
| W54 | 4 | 13.6 | 14.1 | 14 | 13.9 | 12.4 | 12.1 | 12.2 | 12.2 |
| W55 | 4 | 13.9 | 14.2 | 13.8 | 14.0 | 11.7 | 11.6 | 11.9 | 11.7 |
| W6 | 4 | 15 | 15 | 14.4 | 14.8 | 12.1 | 12.2 | 12 | 12.1 |
| W8 | 4 | 14.6 | 14.8 | 15 | 14.8 | 11.6 | 11.8 | 11.7 | 11.7 |
| W86 | 4 | 15.1 | 15.7 | 16.4 | 15.7 | 13.1 | 14 | 13.7 | 13.6 |
| W87 | 4 | 14.1 | 14.4 | 14.3 | 14.3 | 12.7 | 12.3 | 12.1 | 12.4 |
| W88 | 4 | 13.3 | 13.1 | 14.2 | 13.5 | 11.9 | 11.9 | 12.1 | 12.0 |
| W9 | 4 | 14.5 | 14.8 | 14.8 | 14.7 | 11.8 | 11.9 | 12.2 | 12.0 |
| Wanfeng505 | 2 | 13.9 | 13.4 | 14.1 | 13.8 | 10.8 | 11 | 11.1 | 11.0 |
| Wanke2mai1720 | - | 13.9 | 14.6 | 14.1 | 14.2 | 11.2 | 11 | 11.4 | 11.2 |
| Wanke800 | 2 | 13.7 | 14.3 | 13.5 | 13.8 | 11.6 | 12.3 | 12.2 | 12.0 |
| Wansu1617 | 2 | 14.6 | 13.9 | 15.3 | 14.6 | 13 | 12.9 | 13.1 | 13.0 |
| Wansu21 | 1 | 15.5 | 16.6 | 16.1 | 16.1 | 11.5 | 11.7 | 11.6 | 11.6 |
| Xianmai283 | 3 | 13.1 | 12.7 | 13 | 12.9 | 13.4 | 13.1 | 12.7 | 13.1 |
| Xiansheng369 | 1 | 13.9 | 14.4 | 14.2 | 14.2 | 12.1 | 12.3 | 13 | 12.5 |
| Xinkemai176 | 2 | 14.7 | 15.1 | 15.1 | 15.0 | 11.6 | 11.7 | 12 | 11.8 |
| Xinkemai186 | 2 | 15.8 | 16.5 | 15.7 | 16.0 | 11.7 | 12 | 11.7 | 11.8 |
| Xinliang16 | 3 | 13.2 | 12.7 | 12.5 | 12.8 | 11.4 | 10.9 | 11.4 | 11.2 |
| Xinmai26 | 3 | 15.1 | 14.8 | 14.9 | 14.9 | 12.1 | 11.8 | 12.1 | 12.0 |
| Xinmai45 | 2 | 16.1 | 16.6 | 16.8 | 16.5 | 10.5 | 11.3 | 11.5 | 11.1 |
| Xinmai52 | 2 | 13.7 | 14 | 14.1 | 13.9 | 12.2 | 12.4 | 11.9 | 12.2 |
| Xinmai57 | 1 | 14.3 | 13.7 | 13.8 | 13.9 | 11.5 | 11.4 | 11.5 | 11.5 |
| Xinmai58 | 2 | 16.7 | 15.7 | 15.7 | 16.0 | 12.1 | 12.4 | 12.2 | 12.2 |
| Xinmai65 | 2 | 13.9 | 15.5 | 14.9 | 14.8 | 11.2 | 11.6 | 11.6 | 11.5 |
| Xinmai66 | 2 | 14.5 | 14.2 | 15 | 14.6 | 10.7 | 10.8 | 10.9 | 10.8 |
| Xinmai67 | 3 | 14.3 | 14.7 | 14.3 | 14.4 | 13.2 | 14 | 13.3 | 13.5 |
| Xinmai72 | 1 | 14 | 14.6 | 14.9 | 14.5 | 11.5 | 11.7 | 11.8 | 11.7 |
| Xinmai78 | 3 | 14.9 | 14.9 | 15.7 | 15.2 | 11 | 11.9 | 11.4 | 11.4 |
| Xinong1125 | 3 | 15.9 | 16 | 16 | 16.0 | 12.2 | 11.7 | 12.6 | 12.2 |
| Xinong1152 | 1 | 15.4 | 14.5 | 15.9 | 15.3 | 12.9 | 12.3 | 12.2 | 12.5 |
| Xinong1155 | 3 | 14.8 | 14.7 | 15.5 | 15.0 | 12.4 | 12.3 | 12.7 | 12.5 |
| Xinong1522 | 3 | 16.3 | 16.7 | 16.9 | 16.6 | 11.7 | 11.7 | 11.9 | 11.8 |
| Xinong158 | 1 | 14.4 | 15.2 | 15.3 | 15.0 | 11.8 | 11.8 | 11.7 | 11.8 |
| Xinong162 | 1 | 16 | 15.8 | 15.8 | 15.9 | 11.8 | 12.2 | 11.8 | 11.9 |
| Xinong1668 | 3 | 14.5 | 14.3 | 15.3 | 14.7 | 12 | 12.3 | 12.1 | 12.1 |
| Xinong1871 | 3 | 14 | 14.1 | 15.1 | 14.4 | 12.8 | 12.1 | 12.2 | 12.4 |
| Xinong20 | 1 | 16.6 | 15.9 | 15.5 | 16.0 | 11 | 11.5 | 11.2 | 11.2 |
| Xinong301 | 1 | 14.1 | 14.3 | 14 | 14.1 | 10.3 | 10.3 | 10.5 | 10.4 |
| Xinong5189 | 3 | 15.1 | 15.4 | 15.4 | 15.3 | 12.8 | 13.3 | 13.3 | 13.1 |
| Xinong5195 | 3 | 15.3 | 17.2 | 16.2 | 16.2 | 10.9 | 11.4 | 11 | 11.1 |
| Xinong579 | 3 | 15.9 | 16.6 | 15.4 | 16.0 | 12.9 | 12.2 | 13.1 | 12.7 |
| Xinong586 | 1 | 13.9 | 14.1 | 14.3 | 14.1 | 11.6 | 11.1 | 11.4 | 11.4 |
| Xinong633 | 2 | 14.9 | 14.7 | 14.5 | 14.7 | 10.9 | 10.5 | 10.3 | 10.6 |
| Xinong635 | 2 | 15.9 | 15.2 | 16.3 | 15.8 | 11.6 | 11.3 | 11.5 | 11.5 |
| Xinong805a | 1 | 16.2 | 15.4 | 16.5 | 16.0 | 11.5 | 12 | 12 | 11.8 |
| Xinong839 | 1 | 15.5 | 16.6 | 16.7 | 16.3 | 12.7 | 13.2 | 12.8 | 12.9 |
| Xinong857 | 2 | 14.6 | 14.8 | 14.6 | 14.7 | 11.5 | 11.5 | 10.8 | 11.3 |
| Xinong867 | 1 | 14.6 | 13.9 | 14.5 | 14.3 | 11.4 | 11.7 | 11.4 | 11.5 |
| Xinong9198 | 3 | 17 | 16.6 | 17.6 | 17.1 | 12.1 | 12.1 | 12.1 | 12.1 |
| Xinong926 | 1 | 13.2 | 13.7 | 13.6 | 13.5 | 12.4 | 13.4 | 12.5 | 12.8 |
| Xinong962 | 3 | 13.7 | 14.4 | 14.4 | 14.2 | 11.7 | 11.9 | 12.5 | 12.0 |
| Xinong963 | 1 | 14.9 | 15 | 15.2 | 15.0 | 12.4 | 12.3 | 12.7 | 12.5 |
| Xinong9799 | - | 15.8 | 15.6 | 16.5 | 16.0 | 11.1 | 11.6 | 11.5 | 11.4 |
| Xinong9866 | - | 14.1 | 14.3 | 13.8 | 14.1 | 11.9 | 12.4 | 12.3 | 12.2 |
| Xinshiji2hao | - | 13.2 | 14 | 13.7 | 13.6 | 11.8 | 12.4 | 12.6 | 12.3 |
| Xuke108 | 2 | 15.4 | 15.2 | 14.6 | 15.1 | 13.3 | 13.2 | 12.8 | 13.1 |
| Xuke13 | 1 | 15.1 | 14.9 | 14.5 | 14.8 | 12.3 | 12.4 | 13 | 12.6 |
| Xuke16 | 3 | 14.7 | 14.9 | 14.7 | 14.8 | 11.1 | 11.4 | 11.3 | 11.3 |
| Xumai17016 | 2 | 14.6 | 13.1 | 13.8 | 13.8 | 12.4 | 12.4 | 12.5 | 12.4 |
| Xumai17106 | 3 | 14.3 | 13.2 | 13.7 | 13.7 | 12 | 11.7 | 12.5 | 12.1 |
| Xumai18197 | 2 | 14.7 | 14.3 | 15.2 | 14.7 | 12.5 | 12.1 | 13 | 12.5 |
| Xumai2198 | 2 | 16.3 | 16 | 16.2 | 16.2 | 12.1 | 11.5 | 12.2 | 11.9 |
| Yanbaol369 | - | 15.6 | 15.9 | 16.1 | 15.9 | 12.3 | 12.6 | 12.5 | 12.5 |
| Yangmai15 | 2 | 13.6 | 12.8 | 13 | 13.1 | 12.7 | 12.2 | 12.5 | 12.5 |
| Yingqiang1hao | 2 | 16.5 | 16.4 | 16.6 | 16.5 | 12.6 | 12.2 | 11.6 | 12.1 |
| Yunong168 | 1 | 15.8 | 15 | 15 | 15.3 | 11.9 | 12 | 11.8 | 11.9 |
| Yunong612 | 1 | 12.7 | 12.5 | 12.9 | 12.7 | 12.2 | 12 | 12.3 | 12.2 |
| Yunong7168 | 1 | 15.5 | 15.6 | 16 | 15.7 | 12.5 | 12.2 | 12.1 | 12.3 |
| Yunong7928 | 2 | 14.8 | 14.7 | 13.6 | 14.4 | 13 | 12.6 | 13.1 | 12.9 |
| Yunong804 | 3 | 12.3 | 12.8 | 12.9 | 12.7 | 11.4 | 11.7 | 11.5 | 11.5 |
| Yunong905 | 3 | 15.2 | 16 | 15.2 | 15.5 | 11.8 | 12 | 11.3 | 11.7 |
| Yunong907 | 2 | 14.7 | 14.7 | 15 | 14.8 | 11.9 | 11.7 | 11.9 | 11.8 |
| Yunong912 | 1 | 15 | 15.2 | 14.4 | 14.9 | 11.6 | 11.6 | 11.9 | 11.7 |
| Yunong917 | 3 | 15.3 | 15.7 | 15.8 | 15.6 | 12.5 | 12.7 | 12.7 | 12.6 |
| Yunong923 | 1 | 14.3 | 14 | 13.8 | 14.0 | 11.8 | 11.7 | 11.3 | 11.6 |
| Yutong120 | 2 | 16 | 16 | 15.9 | 16.0 | 11.5 | 11.7 | 11.6 | 11.6 |
| Yuzhou121 | 2 | 15.4 | 15.4 | 15.2 | 15.3 | 12.3 | 12.7 | 12.6 | 12.5 |
| Yuzhou136 | 3 | 16.5 | 16.6 | 15.5 | 16.2 | 12.9 | 12.9 | 12.5 | 12.8 |
| Zhengda181 | 1 | 13.3 | 13 | 12.9 | 13.1 | 11.2 | 11.5 | 11.6 | 11.4 |
| Zhengda201 | 1 | 14.6 | 13.9 | 13.3 | 13.9 | 12.5 | 12.2 | 12 | 12.2 |
| Zhengmai113 | 2 | 16.3 | 15.7 | 16.1 | 16.0 | 12.6 | 12.3 | 12.9 | 12.6 |
| Zhengmai132 | 1 | 13.4 | 13.7 | 14.2 | 13.8 | 10.9 | 11 | 10.4 | 10.8 |
| Zhengmai136 | 2 | 16.2 | 17 | 17.1 | 16.8 | 11.5 | 11.3 | 11.7 | 11.5 |
| Zhengmai139 | 2 | 15.5 | 15 | 15.4 | 15.3 | 11.6 | 11.4 | 11.2 | 11.4 |
| Zhengmai163 | 2 | 14.1 | 14.2 | 14.3 | 14.2 | 12.9 | 12.6 | 12.5 | 12.7 |
| Zhengmai1831 | 3 | 13.2 | 13.3 | 14.3 | 13.6 | 11.1 | 11.4 | 11.8 | 11.4 |
| Zhengmai1905 | 1 | 13.7 | 12.6 | 13.6 | 13.3 | 12.7 | 12.5 | 12.5 | 12.6 |
| Zhengmai1926 | 1 | 14.5 | 13.9 | 15.3 | 14.6 | 11.4 | 10.9 | 10.8 | 11.0 |
| Zhengmai201 | 1 | 14.4 | 14.5 | 14.4 | 14.4 | 12 | 11.9 | 11.8 | 11.9 |
| Zhengmai2018 | 3 | 14.9 | 15.1 | 15.6 | 15.2 | 11.4 | 11.4 | 11.5 | 11.4 |
| Zhengmai21 | 2 | 13.6 | 14.1 | 13.6 | 13.8 | 11.5 | 11 | 11.3 | 11.3 |
| Zhengmai216 | 2 | 13.9 | 15 | 15.2 | 14.7 | 12.1 | 12.9 | 12.8 | 12.6 |
| Zhengmai22 | 1 | 15.8 | 15.9 | 16 | 15.9 | 12.3 | 12.4 | 12.6 | 12.4 |
| Zhengmai23 | 1 | 14.5 | 13.7 | 13.9 | 14.0 | 12 | 12.4 | 11.8 | 12.1 |
| Zhengmai29 | 1 | 18.4 | 18.4 | 17.5 | 18.1 | 11 | 10.4 | 10.7 | 10.7 |
| Zhengmai366 | 3 | 15.1 | 15.4 | 15 | 15.2 | 10.6 | 10.6 | 11 | 10.7 |
| Zhengmai518 | 2 | 14.5 | 14.3 | 14.2 | 14.3 | 12.3 | 11.8 | 12 | 12.0 |
| Zhengmai6166 | 3 | 14.3 | 14 | 14.3 | 14.2 | 11.6 | 11.4 | 11.9 | 11.6 |
| Zhengmai618 | 1 | 14.9 | 15 | 15.5 | 15.1 | 10.7 | 10.6 | 10.3 | 10.5 |
| Zhengmai823 | 3 | 14.6 | 14.2 | 14.9 | 14.6 | 13.6 | 13.3 | 13.7 | 13.5 |
| Zhengmai825 | 3 | 13.7 | 14.9 | 14.2 | 14.3 | 12.3 | 12.1 | 12.6 | 12.3 |
| Zhengmai826 | 2 | 16 | 15.8 | 16.3 | 16.0 | 11.8 | 11.9 | 11.8 | 11.8 |
| Zhengmai827 | 3 | 14.5 | 14.8 | 14.4 | 14.6 | 11.5 | 11.6 | 11.9 | 11.7 |
| Zhengmai828 | 2 | 14.6 | 15.7 | 15.3 | 15.2 | 11.5 | 11.9 | 11.8 | 11.7 |
| Zhengmai917 | 1 | 14.1 | 14.3 | 14.4 | 14.3 | 11.7 | 10.8 | 11.1 | 11.2 |
| Zhengmai918 | 3 | 14.3 | 15.7 | 15.8 | 15.3 | 11 | 11.7 | 11.7 | 11.5 |
| Zhengmai9699 | 1 | 17.2 | 17.3 | 16.7 | 17.1 | 13.4 | 13.5 | 12.8 | 13.2 |
| Zhengpinmai25 | 1 | 14.1 | 14 | 13.3 | 13.8 | 12.1 | 11.8 | 11.8 | 11.9 |
| Zhengshimai9170 | - | 14.2 | 14.2 | 13.6 | 14.0 | 11.2 | 11.3 | 10.7 | 11.1 |
| Zhengyanmai182 | 1 | 13.7 | 13.9 | 13.8 | 13.8 | 12.7 | 12.2 | 12.5 | 12.5 |
| Zhongmai255 | 2 | 16.1 | 16 | 16.4 | 16.2 | 10.9 | 10.7 | 10.7 | 10.8 |
| Zhongmai6032 | 2 | 14.1 | 14.3 | 14 | 14.1 | 12.7 | 12.3 | 12 | 12.3 |
| Zhongmai6301 | 2 | 15.2 | 15.7 | 15.3 | 15.4 | 10.7 | 11.1 | 10.9 | 10.9 |
| Zhongmai698 | 1 | 14.8 | 15.3 | 15.3 | 15.1 | 10.9 | 11.2 | 11.4 | 11.2 |
| Zhongnong031 | 2 | 14.5 | 15.5 | 15.3 | 15.1 | 11.7 | 10.9 | 11.2 | 11.3 |
| Zhongnong539 | 3 | 13.5 | 13.2 | 13.4 | 13.4 | 12 | 11.6 | 11.6 | 11.7 |
| Zhongyan270 | 1 | 13.8 | 13.3 | 14.6 | 13.9 | 11.1 | 10.9 | 11.5 | 11.2 |
| Zhongyu049 | 3 | 16.1 | 16.3 | 15.6 | 16.0 | 11.2 | 11.4 | 11.2 | 11.3 |
| Zhongyu1211 | 3 | 14.2 | 14.3 | 14.5 | 14.3 | 12.7 | 12.4 | 12.7 | 12.6 |
| Zhongyu1220 | 1 | 14.7 | 15.3 | 15.5 | 15.2 | 12.1 | 11.8 | 11.6 | 11.8 |
| Zhongyu130 | 3 | 15.8 | 16.2 | 16.2 | 16.1 | 10.5 | 10.6 | 10.6 | 10.6 |
| Zhongyu149 | 3 | 14.9 | 14.9 | 14.9 | 14.9 | 12 | 12 | 12.3 | 12.1 |
| Zhongyu1702 | 1 | 15 | 15.2 | 15.3 | 15.2 | 12 | 11.8 | 12 | 11.9 |
| Zhongyu36 | - | 15 | 14.4 | 15.2 | 14.9 | 11.4 | 10.9 | 11.3 | 11.2 |
| Zhongyu978 | 1 | 17.3 | 17.4 | 17.3 | 17.3 | 12.2 | 12.1 | 12 | 12.1 |
| Zhongyu980 | 1 | 16.2 | 16 | 16.2 | 16.1 | 10.9 | 10.8 | 10.8 | 10.8 |
| Zhongyuan26 | 1 | 17.2 | 16.6 | 16.3 | 16.7 | 12.6 | 12.1 | 12 | 12.2 |
| Zhongyuanfeng1hao | 1 | 16.4 | 17.8 | 15.8 | 16.7 | 11.6 | 12.1 | 11.8 | 11.8 |
| Zhongzhimai13 | 1 | 14.8 | 13.9 | 14.6 | 14.4 | 13.2 | 12.4 | 12.8 | 12.8 |
| Zhongzhimai22 | 3 | 13.9 | 14.1 | 13 | 13.7 | 10.4 | 11.5 | 10.8 | 10.9 |
| Zhongzhu16 | - | 17.2 | 16.9 | 16.8 | 17.0 | 12.9 | 12.5 | 12.8 | 12.7 |
| Zhoumai18 | 1 | 14.8 | 14.4 | 14.5 | 14.6 | 11.6 | 12.3 | 12.3 | 12.1 |
| Zhoumai22 | 1 | 14.5 | 15.3 | 14.9 | 14.9 | 11.3 | 11.4 | 11.1 | 11.3 |
| Zhoumai36 | 1 | 14.8 | 15.3 | 14.7 | 14.9 | 12.3 | 13 | 12.4 | 12.6 |
| Zhoumai48 | 1 | 15.6 | 16.5 | 15.9 | 16.0 | 11.9 | 12.2 | 12.4 | 12.2 |
| Zhoumai52hao | 1 | 16 | 16.1 | 16.3 | 16.1 | 10.4 | 10.9 | 10.8 | 10.7 |
| Zhumai562 | 1 | 13.1 | 14.5 | 13.4 | 13.7 | 11.2 | 11.9 | 11.6 | 11.6 |
| Zhumai566 | 1 | 13.7 | 14.1 | 14 | 13.9 | 10.9 | 10.7 | 11.1 | 10.9 |
| Zhumai567 | 2 | 14.6 | 15 | 14.4 | 14.7 | 12.2 | 11.8 | 12.1 | 12.0 |
| Zhumai568 | 1 | 16.3 | 15.9 | 16 | 16.1 | 11.6 | 11.8 | 11.8 | 11.7 |
| Zhumai569 | 3 | 14.7 | 14.3 | 14.2 | 14.4 | 11.9 | 11.8 | 11.8 | 11.8 |
| Zhumai586 | 2 | 14.5 | 15.1 | 14.6 | 14.7 | 11 | 11.6 | 11 | 11.2 |
| Zhumai591 | 1 | 13.7 | 13.6 | 14 | 13.8 | 12.3 | 12.1 | 12.7 | 12.4 |
| Zhumai592 | 1 | 15.3 | 15.2 | 15.6 | 15.4 | 11.4 | 11.4 | 11.6 | 11.5 |
| Zhumai596 | 1 | 14.5 | 14.3 | 14.2 | 14.3 | 12.9 | 12.2 | 12.6 | 12.6 |
| Zhumai598 | 1 | 13.2 | 12.7 | 13.2 | 13.0 | 10.7 | 10.8 | 11.5 | 11.0 |
| Zhumai599 | 3 | 14.1 | 14.4 | 13.6 | 14.0 | 12.6 | 12.5 | 12 | 12.4 |
| Zhumai726 | 2 | 15.8 | 15.7 | 15.4 | 15.6 | 11.8 | 12 | 11.3 | 11.7 |
| Zhumai762 | 3 | 14.6 | 15 | 14.3 | 14.6 | 11.3 | 11.6 | 11.9 | 11.6 |
| Sample Group | Skewness | Kurtosis | JB Statistic | p-Value | Conforms to Normal Distribution? |
|---|---|---|---|---|---|
| E1 | 0.003 | 3.129 | 0.372 | 0.830 | Yes |
| E2 | 0.102 | 3.107 | 0.466 | 0.792 | Yes |
| E3 | −0.003 | 3.168 | 0.656 | 0.720 | Yes |
| E4 | 0.035 | 3.149 | 0.377 | 0.828 | Yes |
| E5 | 0.097 | 2.970 | 0.359 | 0.836 | Yes |
| E6 | 0.080 | 2.937 | 0.542 | 0.763 | Yes |
| E7 | −0.006 | 3.076 | 0.307 | 0.858 | Yes |
| E8 | 0.059 | 3.038 | 0.177 | 0.915 | Yes |
| Source of Variation | Df | SS | MS | F-Value | p-Value | ||||
|---|---|---|---|---|---|---|---|---|---|
| GPC | WGC | GPC | WGC | GPC | WGC | GPC | WGC | ||
| Genotypes | 309 | 2304.1 | 4079.2 | 7.46 | 13.2 | 15.12 | 23.3 | <0.01 | <0.01 |
| Environments | 3 | 205,757.2 | 497,393.1 | 68,585.0 | 165,797.0 | 417,174.67 | 876,285 | <0.01 | <0.01 |
| Replicates (environments) | 2 | 0.9 | 2.2 | 0.5 | 1.1 | 0.91 | 1.9 | 0.4 | 0.14 |
| GenotypeEnvironment | 927 | 324.1 | 1924.0 | 1.1 | 2.1 | 2.13 | 11.0 | <0.01 | <0.01 |
| Error | 247 | ||||||||
| Chromosome | No. of the Marker | Physical Length (Mb) | Marker Density (Marker/Mb) |
|---|---|---|---|
| 1A | 5156 | 598.6 | 8.6 |
| 2A | 6537 | 787.7 | 8.3 |
| 3A | 5606 | 754.0 | 7.4 |
| 4A | 5297 | 754.2 | 7.0 |
| 5A | 5733 | 713.3 | 8.0 |
| 6A | 4905 | 622.6 | 7.9 |
| 7A | 5676 | 744.5 | 7.6 |
| 1B | 4777 | 700.3 | 6.8 |
| 2B | 6541 | 812.7 | 8.0 |
| 3B | 6173 | 851.9 | 7.2 |
| 4B | 4659 | 673.6 | 6.9 |
| 5B | 5908 | 714.8 | 8.3 |
| 6B | 5284 | 731.1 | 7.2 |
| 7B | 5581 | 763.7 | 7.3 |
| 1D | 3931 | 498.6 | 7.9 |
| 2D | 5270 | 656.4 | 8.0 |
| 3D | 4703 | 619.5 | 7.6 |
| 4D | 3568 | 518.2 | 6.9 |
| 5D | 4755 | 569.8 | 8.3 |
| 6D | 3725 | 495.3 | 7.5 |
| 7D | 5051 | 642.8 | 7.9 |
| A | 38,910 | 4974.7 | 7.8 |
| B | 38,923 | 5248.0 | 7.4 |
| D | 31,003 | 4000.6 | 7.7 |
| ALL | 108,836 | 14,223.3 | 7.7 |
| Name | Kasp-GPC-3AL | Kasp-GPC-3BL | Kasp-GPC-4BL | Kasp-WGC-5AL | Kasp-WGC-5DS | WGC (%) | GPC (%) |
|---|---|---|---|---|---|---|---|
| Huaimai20 | GG | CC | CC | AA | GG | 31.6 | 14.4 |
| Huaimai18 | GG | CC | CC | AA | AA | 32.4 | 14.5 |
| Lumai21 | AA | CC | CC | GG | AA | 34.2 | 15.3 |
| Wanmai38 | AA | CC | CC | GG | AA | 33.8 | 15.5 |
| Wennong5 | AA | CC | CC | GG | AA | 34.3 | 15.3 |
| Jinmai61 | AA | CC | CC | AA | AA | 32.1 | 14.3 |
| Xinong1376 | AA | TT | CC | AA | AA | 33.2 | 15.1 |
| Yumai7 | AA | TT | CC | GG | AA | 35.6 | 16.6 |
| Fengchan3 | AA | CC | CC | AA | AA | 32.7 | 14.1 |
| Jimai20 | GG | CC | CC | GG | AA | 32.4 | 13.9 |
| Lumai6 | GG | CC | CC | AA | GG | 29.7 | 13.7 |
| Shiyou17 | AA | CC | CC | GG | AA | 34.4 | 15.5 |
| Su0663 | GG | CC | CC | AA | GG | 29.7 | 12.9 |
| Wanmai53 | GG | CC | CC | AA | GG | 31.6 | 14.1 |
| Lankao23 | AA | TT | CC | AA | AA | 32.8 | 14.9 |
| Linkang12 | AA | CC | CC | GG | AA | 35.8 | 16.1 |
| Luyuan502 | AA | CC | CC | AA | GG | 31.3 | 14.1 |
| Neixiang188 | AA | CC | CC | AA | GG | 33.7 | 15.9 |
| Shi4185 | GG | CC | CC | AA | GG | 32.0 | 14.8 |
| Shijiazhuang15 | AA | CC | CC | AA | AA | 32.7 | 14.5 |
| Shijiazhuang8 | AA | CC | CC | AA | GG | 31.6 | 14.5 |
| Xinong2000-7 | AA | TT | CC | AA | AA | 33.4 | 14.8 |
| Xinong291 | AA | CC | CC | AA | AA | 33.3 | 15.4 |
| Yumai13 | GG | CC | CC | AA | AA | 32.2 | 15.1 |
| Yumai35 | GG | TT | CC | AA | GG | 32.5 | 15.2 |
| Zhongmai871 | GG | CC | CC | GG | GG | 33.6 | 15.2 |
| Zhongmai875 | GG | TT | CC | GG | AA | 34.3 | 14.7 |
| Zhongmai895 | GG | CC | CC | GG | AA | 34.8 | 14.7 |
| Zhongyu9 | AA | TT | CC | AA | GG | 30.7 | 14.2 |
| Shannong20 | AA | CC | CC | AA | AA | 28.5 | 12.8 |
| Shan150 | AA | CC | CC | GG | GG | 34.8 | 16.3 |
| Taishan5 | AA | CC | CC | GG | AA | 34.1 | 14.6 |
| Wanmai29 | GG | CC | CC | AA | GG | 31.7 | 13.3 |
| Wennong14 | AA | CC | CC | AA | AA | 32.7 | 14.0 |
| Yannong15 | AA | CC | CC | AA | AA | 32.6 | 14.4 |
| Yannong19 | AA | CC | CC | AA | AA | 33.7 | 14.3 |
| Huapei5 | AA | CC | CC | AA | GG | 30.8 | 13.0 |
| Yannong18 | AA | CC | CC | AA | GG | 31.1 | 13.9 |
| Zhoumai13 | AA | TT | CC | GG | AA | 32.8 | 15.0 |
| Zhoumai30 | AA | CC | CC | GG | GG | 31.2 | 13.1 |
| Yumai57 | GG | CC | CC | GG | GG | 29.4 | 13.0 |
| Zhoumai19 | GG | CC | CC | AA | AA | 32.0 | 14.6 |
| Zhoumai31 | AA | CC | CC | AA | GG | 31.6 | 14.0 |
| Zhengmai366 | AA | CC | CC | AA | AA | 30.8 | 15.5 |
| Lumai14 | GG | CC | CC | GG | AA | 33.5 | 14.5 |
| Jinan17 | GG | CC | CC | GG | AA | 35.0 | 12.9 |
| Lumai9 | GG | CC | CC | AA | GG | 30.5 | 13.5 |
| Xinong979-005 | AA | CC | CC | AA | AA | 33.5 | 14.7 |
| Shan715 | GG | CC | CC | AA | GG | 31.3 | 13.6 |
| Wunong148 | GG | TT | CC | AA | GG | 29.9 | 13.2 |
| Yumai50 | AA | CC | CC | AA | AA | 32.1 | 14.2 |
| Xinmai9408 | GG | CC | CC | AA | GG | 32.0 | 13.9 |
| Bima4 | GG | TT | CC | GG | GG | 31.5 | 13.6 |
| Linmai2 | AA | TT | CC | GG | AA | 36.3 | 16.0 |
| Jishi02-1 | AA | CC | CC | AA | AA | 35.2 | 14.1 |
| Shanmai509 | AA | CC | CC | GG | AA | 33.0 | 14.1 |
| Shan512 | AA | TT | CC | GG | AA | 36.9 | 16.0 |
| Sunong6 | AA | CC | CC | GG | GG | 35.6 | 16.1 |
| Wanmai33 | AA | TT | CC | GG | GG | 35.7 | 15.9 |
| Zhoumai28 | AA | TT | CC | GG | GG | 34.7 | 15.2 |
| Gaoyou503 | AA | CC | CC | AA | GG | 34.6 | 15.1 |
| Bima1 | AA | TT | NA | GG | NA | 33.2 | 15.1 |
| Heng7228 | AA | CC | NA | AA | NA | 31.6 | 14.8 |
| Huaimai21 | AA | TT | NA | AA | NA | 31.9 | 15.0 |
| Jimai21 | AA | TT | NA | AA | NA | 33.5 | 15.1 |
| Jinhe9123 | AA | CC | NA | AA | NA | 32.9 | 15.0 |
| Zhoumai16 | AA | CC | NA | GG | NA | 31.6 | 14.0 |
| Zhoumai22 | AA | CC | NA | AA | NA | 31.3 | 14.3 |
| Fu936 | AA | CC | NA | AA | NA | 31.6 | 14.6 |
| Gaocheng8901 | AA | CC | NA | AA | NA | 33.6 | 14.7 |
| Jimai22 | AA | CC | NA | AA | NA | 32.3 | 14.4 |
| Jinan13 | AA | CC | NA | AA | NA | 31.4 | 14.2 |
| Liangxing66 | AA | CC | NA | AA | NA | 30.7 | 13.7 |
| Liangxing99 | AA | CC | NA | AA | NA | 30.0 | 13.7 |
| Linhan2 | GG | CC | NA | AA | NA | 28.6 | 13.6 |
| Yumai63 | AA | CC | NA | AA | NA | 30.1 | 13.5 |
| Zheng9023 | AA | CC | NA | AA | NA | 31.2 | 13.7 |
| Zhengyin1 | AA | CC | NA | AA | NA | 30.1 | 13.2 |
| Lumai5 | AA | CC | NA | AA | NA | 34.0 | 16.0 |
| Neixiang5 | AA | CC | NA | AA | NA | 33.1 | 13.7 |
| Zhengzhou3 | AA | CC | NA | GG | NA | 32.7 | 14.4 |
| Shixin733 | AA | CC | NA | AA | NA | 31.1 | 13.2 |
| Wanmai52 | AA | CC | NA | AA | NA | 32.5 | 13.5 |
| Wanmai19 | AG | CC | NA | AA | NA | 31.9 | 14.3 |
| Linmai4 | GG | CC | NA | AA | NA | 30.7 | 13.3 |
| Shan229 | AA | CC | NA | GG | NA | 34.9 | 15.2 |
| Taishan1 | AA | TT | NA | GG | NA | 35.3 | 15.2 |
| Xinong88 | AA | CC | NA | AA | NA | 32.9 | 14.5 |
| Yumai34 | AA | TT | NA | AA | NA | 34.4 | 15.1 |
| Shan354 | GG | TT | NA | AA | NA | 34.6 | 14.6 |
| Zhoumai18 | GG | CC | NA | GG | NA | 32.1 | 13.6 |
| Shan253 | GG | CC | NA | AA | NA | 31.9 | 13.7 |
| Shixin828 | AA | CC | TT | AA | GG | 31.4 | 13.6 |
| Lumai11 | AA | CC | TT | AA | GG | 31.0 | 14.1 |
| Luami15 | GG | CC | TT | AA | GG | 30.8 | 14.1 |
| Lumai8 | AA | CC | TT | AA | GG | 31.3 | 14.3 |
| Wanmai50 | AA | TT | TT | GG | AA | 33.5 | 15.0 |
| Lankao906 | AA | CC | TT | AA | AA | 31.9 | 14.5 |
| Lankao24 | AA | CC | TT | AA | AA | 32.4 | 14.4 |
| Shannong78-59 | AA | CC | TT | AA | GG | 33.0 | 14.7 |
| Zhongyu5 | AG | TT | TT | AA | GG | 30.8 | 13.6 |
| Zhoumai11 | AA | CC | TT | GG | GG | 34.3 | 14.7 |
| Lumai23 | AA | CC | TT | AA | AA | 32.6 | 13.9 |
| Luohan2 | GG | CC | TT | AA | AA | 31.1 | 13.7 |
| Shannong981 | AA | TT | TT | AA | AA | 31.0 | 13.4 |
| Yanzhan4110 | AA | CC | TT | GG | GG | 29.3 | 15.2 |
| Aikang58 | GG | CC | TT | AA | GG | 29.4 | 12.6 |
| Luomai21 | AA | CC | TT | AA | GG | 31.9 | 13.8 |
| Zhou8425B | AA | CC | TT | GG | GG | 30.0 | 13.3 |
| Bainong64 | GG | CC | TT | GG | GG | 30.9 | 13.1 |
| Wan23094 | AA | CC | TT | GG | GG | 30.9 | 13.0 |
| Yumai47 | GG | CC | TT | AA | GG | 30.9 | 13.7 |
| Yumai49 | GG | CC | TT | GG | GG | 27.3 | 12.3 |
| Jimai19 | GG | CC | TT | GG | GG | 30.4 | 12.7 |
| Shanmai94 | AA | CC | TT | AA | GG | 30.3 | 13.3 |
| Han6172 | AA | CC | TT | AA | GG | 27.8 | 11.8 |
| Hengguan33 | GG | CC | TT | AA | AA | 32.6 | 14.9 |
| Zhong892 | AA | CC | TT | GG | AA | 32.9 | 13.6 |
| Jining16 | GG | CC | TT | AA | AA | 31.3 | 13.1 |
| Zhoumai12 | AA | CC | TT | GG | AA | 33.6 | 14.3 |
| Shanyou225 | GG | CC | TT | GG | AA | 34.6 | 13.4 |
| Xinmai9 | AA | CC | TT | AA | GG | 33.0 | 14.3 |
| Lumai7 | AA | CC | TT | AA | GG | 32.2 | 14.8 |
References
- Rasheed, A.; Liu, J.; Appels, R.; He, Z. Mobilizing Triticeae diversity from gene banks to farmer’s field. Mol. Plant 2025, 18, 566–569. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- He, Z.; Xia, X.; Chen, X.; Zhuang, Q. Progress of wheat breeding in China and the future perspective. Acta Agron. Sin. 2011, 37, 202–215. [Google Scholar] [CrossRef] [Scilit]
- Guo, H.Y.; Liu, Y.J.; Yuan, S.H.; Yue, J.R.; Li, Y.M.; Liao, X.Z.; Ying, S.K.; Liu, Z.H.; Bai, J.F.; Zhang, L.P. Superoxide dismutase promotes early flowering in Triticum aestivum L. Agric. Commun. 2023, 1, 100007. [Google Scholar] [CrossRef] [Scilit]
- Ma, M.; Li, Y.; Xue, C.; Xiong, W.; Peng, Z.; Han, X.; Ju, H.; He, Y. Current situation and key parameters for improving wheat quality in China. Front. Plant Sci. 2021, 12, 638525. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; Li, B. Detection of the spatio-temporal differentiation patterns and influencing factors of wheat production in Huang-Huai-Hai region. Foods 2022, 11, 1617. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Q.J.; Wu, D.L.; Gao, J. Variation of winter wheat phenology dataset in Huang Huai Hai Plain of China from 1981 to 2021. Sci. Data 2025, 12, 1203. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Meng, E.; Loyns, A.; Peña, R.J. Wheat quality in the developing world: Trends and opportunities. In Wheat Facts and Futures; Dixon, J., Braun, H.-J., Kosina, P., Crouch, J., Eds.; CIMMYT: El Batán, Mexico, 2009; pp. 24–33. [Google Scholar]
- Zhao, J.; Sun, L.; Hu, M.; Liu, Q.; Xu, J.; Mu, L.; Wang, J.; Yang, J.; Wang, P.; Li, Q.; et al. Pleiotropic quantitative trait loci (QTL) mining for regulating wheat processing quality- and yield-related traits. Plants 2024, 13, 2545. [Google Scholar] [CrossRef] [Scilit]
- Alemu, A.; El Baouchi, A.; El Hanafi, S.; Kehel, Z.; Eddakhir, K.; Tadesse, W. Genetic analysis of grain protein content and dough quality traits in elite spring bread wheat (Triticum aestivum) lines through association study. J. Cereal Sci. 2021, 100, 103214. [Google Scholar] [CrossRef] [Scilit]
- Li, N.; Miao, Y.; Ma, J.; Zhang, P.; Chen, T.; Liu, Y.; Che, Z.; Shahinnia, F.; Yang, D. Consensus genomic regions for grain quality traits in wheat revealed by Meta-QTL analysis and in silico transcriptome integration. Plant Genome 2023, 16, e20336. [Google Scholar] [CrossRef] [Scilit]
- Khalid, A.; Hameed, A.; Tahir, M.F. Wheat quality: A review on chemical composition, nutritional attributes, grain anatomy, types, classification, and function of seed storage proteins in bread making quality. Front. Nutr. 2023, 10, 1053196. [Google Scholar] [CrossRef] [Scilit]
- Pu, Z.; Ye, X.; Li, Y.; Shi, B.; Guo, Z.; Dai, S.; Ma, J.; Liu, Z.; Jiang, Y.; Li, W.; et al. Identification and validation of novel loci associated with wheat quality through a genome-wide association study. J. Integr. Agric. 2022, 21, 3131–3147. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Lai, X.; Chen, Y.; Zhao, P.; Wang, X.; Ji, W.; Xu, S. Selection and application of four QTL for grain protein content in modern wheat cultivars. J. Integr. Agric. 2024, 23, 2557–2570. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Han, J.; Zhang, T.; Sun, M.; Ren, H.; Bo, C.; Diao, Y.; Ma, X.; Wang, H.; Wang, X. Identification and fine mapping of a major QTL, qGPC4D, for grain protein content using wheat-Aegilops tauschii introgression lines. J. Integr. Agric. 2024, 23, 2645–2657. [Google Scholar] [CrossRef] [Scilit]
- Li, Z.; Li, X.; Liu, S.; Mai, S.; Qin, Y.; Wang, S.; Zhou, Z.; Yang, K.; Huang, X.; Deng, Y.; et al. Identification and validation of quantitative trait loci for seven quality-related traits in common wheat (Triticum aestivum L.). Theor. Appl. Genet. 2025, 138, 57. [Google Scholar] [CrossRef] [Scilit]
- Monaghan, J.M.; Snape, J.W.; Chojecki, A.J.S.; Kettlewell, P.S. The use of grain protein deviation for identifying wheat cultivars with high grain protein concentration and yield. Euphytica 2001, 122, 309–317. [Google Scholar] [CrossRef] [Scilit]
- Gao, L.; Meng, C.; Yi, T.; Xu, K.; Cao, H.; Zhang, S.; Yang, X.; Zhao, Y. Genome-wide association study reveals the genetic basis of yield- and quality-related traits in wheat. BMC Plant Biol. 2021, 21, 144. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gudi, S.; Saini, D.K.; Singh, G.; Halladakeri, P.; Kumar, P.; Shamshad, M.; Tanin, M.J.; Singh, S.; Sharma, A. Unravelling consensus genomic regions associated with quality traits in wheat using meta-analysis of quantitative trait loci. Planta 2022, 255, 115. [Google Scholar] [CrossRef] [Scilit]
- Wu, Z.; Qiu, H.; Tian, Z.; Liu, C.; Qin, M.; Li, W.; Yang, P.; Wen, Y.; Tian, B.; Wei, F.; et al. Uncovering the genetic basis of gluten aggregation parameters by genome-wide association analysis in wheat (Triticum aestivum L.) using GlutoPeak. BMC Plant Biol. 2022, 22, 493. [Google Scholar] [CrossRef] [Scilit]
- Hemery, Y.; Rouau, X.; Lullien-Pellerin, V.; Barron, C.; Abecassis, J. Dry processes to develop wheat fractions and products with enhanced nutritional quality. J. Cereal Sci. 2007, 46, 327–347. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Zhou, Y.; Xin, W.; Wei, Y.; Zhang, J.; Guo, L. Wheat breeding in northern China: Achievements and technical advances. Crop J. 2019, 7, 718–729. [Google Scholar] [CrossRef] [Scilit]
- Xu, K.; Zhang, Z.; Tian, W.; Zhi, L.; Yan, J.; Yan, J.; Zheng, C.; Zhang, Y.; Zhang, Y.; He, Z. Comparative analysis of yield and quality traits in two elite Chinese wheat varieties under varied nitrogen fertilizations and environmental conditions. Cereal Chem. 2024, 101, 1139–1149. [Google Scholar] [CrossRef] [Scilit]
- Sandhu, K.S.; Mihalyov, P.D.; Lewien, M.J.; Pumphrey, M.O.; Carter, A.H. Genomic selection and genome-wide association studies for grain protein content stability in a nested association mapping population of wheat. Agronomy 2021, 11, 2528. [Google Scholar] [CrossRef] [Scilit]
- Geyer, M.; Mohler, V.; Hartl, L. Genetics of the inverse relationship between grain yield and grain protein content in common wheat. Plants 2022, 11, 2146. [Google Scholar] [CrossRef] [Scilit]
- Wieser, H.; Koehler, P.; Scherf, K.A. Chemistry of wheat gluten proteins: Quantitative composition. Cereal Chem. 2023, 100, 36–55. [Google Scholar] [CrossRef] [Scilit]
- Law, C.N.; Payne, P.I. Genetical aspects of breeding for improved grain protein content and type in wheat. J. Cereal Sci. 1983, 1, 79–93. [Google Scholar] [CrossRef] [Scilit]
- Shewry, P.R. Improving the protein content and composition of cereal grain. J. Cereal Sci. 2007, 46, 239–250. [Google Scholar] [CrossRef] [Scilit]
- Balyan, H.S.; Gupta, P.K.; Kumar, S.; Dhariwal, R.; Jaiswal, V.; Tyagi, S.; Agarwal, P.; Gahlaut, V.; Kumari, S. Genetic improvement of grain protein content and other health-related constituents of wheat grain. Plant Breed. 2013, 132, 446–457. [Google Scholar] [CrossRef] [Scilit]
- Leonova, I.N.; Kiseleva, A.A.; Berezhnaya, A.A.; Stasyuk, A.I.; Likhenko, I.E.; Salina, E.A. Identification of QTL for grain protein content in Russian spring wheat varieties. Plants 2022, 11, 437. [Google Scholar] [CrossRef] [Scilit]
- Tian, Y.; Liu, P.; Kong, D.; Nie, Y.; Xu, H.; Han, X.; Sang, W.; Li, W. Genome-wide association analysis and KASP markers development for protein quality traits in winter wheat. BMC Plant Biol. 2025, 25, 149. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhou, Z.; Zhang, Z.; Jia, L.; Qiu, H.; Guan, H.; Liu, C.; Qin, M.; Wang, Y.; Li, W.; Yao, W.; et al. Genetic basis of gluten aggregation properties in wheat (Triticum aestivum L.) dissected by QTL mapping of glutopeak parameters. Front. Plant Sci. 2021, 11, 611605. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Leonova, I.N.; Kiseleva, A.A.; Berezhnaya, A.A.; Orlovskaya, O.A.; Salina, E.A. Novel genetic loci from Triticum timopheevii associated with gluten content revealed by GWAS in wheat breeding lines. Int. J. Mol. Sci. 2023, 24, 13304. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Crossa, J.; Pérez-Rodríguez, P.; Cuevas, J.; Montesinos-López, O.; Jarquín, D.; de los Campos, G.; Burgueño, J.; González-Camacho, J.M.; Pérez-Elizalde, S.; Beyen, Y.; et al. Genomic selection in plant breeding: Methods, models, and perspectives. Trends Plant Sci. 2017, 22, 961–975. [Google Scholar] [CrossRef] [Scilit]
- Korte, A.; Farlow, A. The advantages and limitations of trait analysis with GWAS: A review. Plant Methods 2013, 9, 29. [Google Scholar] [CrossRef] [Scilit]
- Gupta, P.K.; Kulwal, P.L.; Jaiswal, V. Association mapping in plants in the post-GWAS genomics era. Adv. Genet. 2019, 104, 75–154. [Google Scholar] [PubMed]
- Sahito, J.H.; Zhang, H.; Gishkori, Z.G.N.; Ma, C.; Wang, Z.; Ding, D.; Zhang, X.; Tang, J. Advancements and prospects of genome-wide association studies (GWAS) in maize. Int. J. Mol. Sci. 2024, 25, 1918. [Google Scholar] [CrossRef] [Scilit]
- Liu, J.; He, Z.; Rasheed, A.; Wen, W.; Yan, J.; Zhang, P.; Wan, Y.; Zhang, Y.; Xie, C.; Xia, X. Genome-wide association mapping of black point reaction in common wheat (Triticum aestivum L.). BMC Plant Biol. 2017, 17, 220. [Google Scholar] [CrossRef] [Scilit]
- Prasad, M.; Kumar, N.; Kulwal, P.; Röder, M.; Balyan, H.; Dhaliwal, H.; Gupta, P. QTL analysis for grain protein content using SSR markers and validation studies using NILs in bread wheat. Theor. Appl. Genet. 2003, 106, 659–667. [Google Scholar] [CrossRef] [Scilit]
- Kumar, A.; Jain, S.; Elias, E.M.; Ibrahim, M.; Sharma, L.K. An Overview of QTL Identification and Marker-Assisted Selection for Grain Protein Content in Wheat. In Eco-Friendly Agro-Biological Techniques for Enhancing Crop Productivity; Sengar, R., Singh, A., Eds.; Springer: Singapore, 2018; pp. 245–274. [Google Scholar]
- Johnson, M.; Kumar, A.; Oladzad-Abbasabadi, A.; Salsman, E.; Aoun, M.; Manthey, F.A.; Elias, M.A. Association mapping for 24 traits related to protein content, gluten strength, color, cooking, and milling quality using balanced and unbalanced data in durum wheat [Triticum turgidum L. var. durum (desf)]. Front. Genet. 2019, 10, 717. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, J.; Zhang, F.; Zhao, C.; Lv, G.; Sun, C.; Pan, Y.; Guo, X.; Chen, F. Genome-wide association study of six quality traits reveals the association of the TaRPP13L1 gene with flour colour in Chinese bread wheat. Plant Biotechnol. J. 2019, 17, 2106–2122. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ahmed, H.G.M.; Sajjad, M.; Zeng, Y.; Iqbal, M.; Khan, S.H.; Ullah, A.; Akhtar, M.N. Genome-wide association mapping through 90K SNP array for quality and yield attributes in bread wheat against water-deficit conditions. Agriculture 2020, 10, 392. [Google Scholar]
- Ruan, Y.; Yu, B.; Knox, R.E.; Zhang, W.; Singh, A.K.; Cuthbert, R.; Fobert, P.; DePauw, R.; Berraies, S.; Sharpe, A.; et al. Conditional mapping identified quantitative trait loci for grain protein concentration expressing independently of grain yield in Canadian durum wheat. Front. Plant Sci. 2021, 12, 642955. [Google Scholar] [CrossRef] [Scilit]
- Hao, S.; Lou, H.; Wang, H.; Shi, J.; Liu, D.; Baogerile; Tao, J.; Miao, S.; Pei, Q.; Yu, L.; et al. Genome-wide association study reveals the genetic basis of five quality traits in Chinese wheat. Front. Plant Sci. 2022, 13, 835306. [Google Scholar] [CrossRef] [Scilit]
- Alqudah, A.M.; Alomari, D.Z.; Thabet, S.G. Pinpointing the genetic keys to enhanced mineral accumulation in wheat grains toward global nutritional challenges. Cereal Res. Commun. 2025, 53, 733–743. [Google Scholar] [CrossRef] [Scilit]
- Echeverry-Solarte, M.; Kumar, A.; Kianian, S.; Simsek, S.; Alamri, M.S.; Mantovani, E.E.; McClean, P.E.; Deckard, E.L.; Elias, E.; Schatz, B.; et al. New QTL alleles for quality-related traits in spring wheat revealed by RIL population derived from supernumerary × non-supernumerary spikelet genotypes. Theor. Appl. Genet. 2015, 128, 893–912. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fatiukha, A.; Filler, N.; Lupo, I.; Lidzbarsky, G.; Klymiuk, V.; Korol, A.B.; Pozniak, C.; Fahima, T.; Krugman, T. Grain protein content and thousand kernel weight QTL identified in a durum × wild emmer wheat mapping population tested in five environments. Theor. Appl. Genet. 2020, 133, 119–131. [Google Scholar] [CrossRef] [Scilit]
- Jiang, P.; Zhang, P.; Wu, L.; He, Y.; Li, C.; Ma, H.; Zhang, X. Linkage and association mapping and Kompetitive allele-specific PCR marker development for improving grain protein content in wheat. Theor. Appl. Genet. 2021, 134, 3563–3575. [Google Scholar] [CrossRef] [Scilit]
- Luo, J.; Li, Z.; Mo, F.; Liao, Y.; Liu, Y. Removal of superior wheat kernels promotes filling of inferior kernels by changing carbohydrate metabolism and sink strength. Crop J. 2021, 9, 1375–1385. [Google Scholar] [CrossRef] [Scilit]
- Suliman, S.; Alemu, A.; Abdelmula, A.A.; Badawi, G.H.; Al-Abdallat, A.; Tadesse, W. Genome-wide association analysis uncovers stable QTL for yield and quality traits of spring bread wheat (Triticum aestivum) across contrasting environments. Plant Gene 2021, 25, 100269. [Google Scholar] [CrossRef] [Scilit]
- Shen, L.; Luo, G.; Song, Y.; Xu, J.; Ji, J.; Zhang, C.; Gregová, E.; Yang, W.; Li, X.; Sun, J.; et al. A novel NAC family transcription factor SPR suppresses seed storage protein synthesis in wheat. Plant Biotechnol. J. 2020, 18, 992–1007. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tabbita, F.; Pearce, S.; Barneix, A.J. Breeding for increased grain protein and micronutrient content in wheat: Ten years of the GPC-B1 gene. J. Cereal Sci. 2017, 73, 183–191. [Google Scholar] [CrossRef] [Scilit]
- Saini, P.; Sheikh, I.; Saini, D.K.; Mir, R.R.; Dhaliwal, H.S.; Tyagi, V. Consensus genomic regions associated with grain protein content in hexaploidy and tetraploid wheat. Front. Genet. 2022, 13, 1021180. [Google Scholar] [CrossRef] [Scilit]
- Kartseva, T.; Alqudah, A.M.; Aleksandrov, V.; Alomari, D.Z.; Doneva, D.; Arif, M.A.R.; Börner, A.; Misheva, S. Nutritional genomic approach for improving grain protein content in wheat. Foods 2023, 12, 1399. [Google Scholar] [CrossRef] [Scilit]
- Nigro, D.; Gadaleta, A.; Mangini, G.; Colasuonno, P.; Marcotuli, I.; Giancaspro, A.; Giove, S.L.; Simeone, R.; Blanco, A. Candidate genes and genome-wide association study of grain protein content and protein deviation in durum wheat. Planta 2019, 249, 1157–1175. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shewry, P.R.; Popineau, Y.; Lafiandra, D.; Belton, P. Wheat glutenin subunits and dough elasticity: Findings of the EUROWHEAT project. Trends Food Sci. Technol. 2000, 11, 433–441. [Google Scholar] [CrossRef] [Scilit]
- Kristensen, P.S.; Ahmed, J.; Andersen, J.R.; Fabio, C.; Jihad, O.; Janss, L.L.; Jensen, J. Genome-wide association studies and comparison of models and cross-validation strategies for genomic prediction of quality traits in advanced winter wheat breeding lines. Front. Plant Sci. 2018, 9, 69. [Google Scholar]
- Shewry, P.R.; Halford, N.G. Genetics of wheat gluten proteins. Adv. Genet. 2003, 49, 111–184. [Google Scholar] [PubMed]
- Cui, F.; Fan, X.; Chen, M.; Zhang, N.; Zhao, C.; Zhang, W.; Han, J.; Ji, J.; Zhao, X.; Yang, L.; et al. QTL detection for wheat kernel size and quality and the responses of these traits to low nitrogen stress. Theor. Appl. Genet. 2016, 129, 469–484. [Google Scholar] [CrossRef] [Scilit]
- Lou, H.; Zhang, R.; Liu, Y.; Guo, D.; Zhai, S.; Chen, A.; Zhang, Y.; Xie, C.; You, M.; Peng, H.; et al. Genome-wide association study of six quality-related traits in common wheat (Triticum aestivum L.) under two sowing conditions. Theor. Appl. Genet. 2021, 134, 399–418. [Google Scholar] [CrossRef] [Scilit]
- Li, J.; Cui, F.; Ding, A.; Zhao, C.; Wang, X.; Wang, L.; Bao, Y.; Qi, X.; Li, X.; Gao, J.; et al. QTL detection of seven quality traits in wheat using two related recombinant inbred line populations. Euphytica 2012, 183, 207–226. [Google Scholar] [CrossRef] [Scilit]
- Goel, S.; Singh, K.; Singh, B.; Grewal, S.; Dwivedi, N.; Alqarawi, A.A.; Allah, E.F.A.; Ahmad, P.; Singh, N.K. Analysis of genetic control and QTL mapping of essential wheat grain quality traits in a recombinant inbred population. PLoS ONE 2019, 14, e0200669. [Google Scholar] [CrossRef] [Scilit]
- Walter, S.; Kahla, A.; Arunachalam, C.; Perochon, A.; Khan, M.R.; Scofield, S.R.; Doohan, F.M. A wheat ABC transporter contributes to both grain formation and mycotoxin tolerance. J. Exp. Bot. 2015, 66, 2583–2593. [Google Scholar] [CrossRef] [Scilit]
- Kumar, R.R.; Bakshi, S.; Goswami, S.; Kumar, S.; Thimmegowda, V.; Jambhulkar, S.J.; Mishra, G.P.; Rai, G.K.; Kumar, S.N.; Singh, B.; et al. Elucidating the Defence Response of Wheat Mutants Developed for augmenting Terminal Heat Stress Tolerance and Improved Grain-Quality. J. Plant Growth Regul. 2024, 43, 3826–3845. [Google Scholar] [CrossRef] [Scilit]
- King, R.W. Abscisic acid in developing wheat grains and its relationship to grain growth and maturation. Planta 1976, 132, 43–51. [Google Scholar] [CrossRef] [Scilit]
- Kishor, P.B.K.; Tiozon, R.N.; Fernie, A.R.; Sreenivasulu, N. Abscisic acid and its role in the modulation of plant growth, development, and yield stability. Trends Plant Sci. 2022, 27, 1283–1295. [Google Scholar] [CrossRef] [Scilit]
- Zulfiqar, B.; Raza, M.A.S.; Saleem, M.F.; Ali, B.; Aslam, M.U.; Al-Ghamdi, A.A.; Elshikh, M.S.; Hassan, M.U.; Toleikienė, M.; Ahmed, J.; et al. Abscisic acid improves drought resilience, growth, physio-biochemical and quality attributes in wheat (Triticum aestivum L.) at critical growth stages. Sci. Rep. 2024, 14, 20411. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Krishnappa, G.; Khan, H.; Krishna, H.; Devate, N.B.; Kumar, S.; Mishra, C.N.; Parkash, O.; Kumar, S.; Kumar, M.; Mamrutha, H.M.; et al. Genome-wide association study for grain protein, thousand kernel weight, and normalized difference vegetation index in bread wheat (Triticum aestivum L.). Genes 2023, 14, 637. [Google Scholar] [CrossRef] [Scilit]
- Zhao, Y.; Yin, T.; Ran, X.; Liu, W.; Shen, Y.; Guo, H.; Parkash, O.; Kumar, S.; Kumar, M.; Mamrutha, H.M.; et al. Stimulus-responsive proteins involved in multi-process regulation of storage substance accumulation during rice grain filling under elevated temperature. BMC Plant Biol. 2023, 23, 547. [Google Scholar] [CrossRef] [Scilit]
- Guérin, C.; Mouzeyar, S.; Roche, J. The landscape of the genomic distribution and the expression of the F-Box genes unveil genome plasticity in hexaploid wheat during grain development and in response to heat and drought stress. Int. J. Mol. Sci. 2021, 22, 3111. [Google Scholar] [CrossRef] [Scilit]
- Shahi, D.; Guo, J.; Pradhan, S.; Avci, M.; Bai, G.; Khan, J.; Baik, B.-K.; Mergoum, M.; Babar, M.A. Genome-Wide Association Study and Genomic Prediction of Soft Wheat End-Use Quality Traits Under Post-Anthesis Heat-Stressed Conditions. Biology 2024, 13, 962. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Wang, M.; Wang, Y.; Liu, H.; Xi, W.; Seung, D.; Wang, X.; Zhuang, L.; Li, H.; Li, T.; et al. The transcription factor MYB44 suppresses starch synthesis to negatively regulate grain weight and yield in wheat and rice. Mol. Plant 2025, 18, 1193–1209. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Luan, H.; Gao, J.; Qu, X.; Li, Y.; Wu, Y.; Wang, J.; Li, S.; Xu, M.; Xu, X.; Sun, M.; et al. Integrating genome-wide association and whole transcriptome analysis to reveal genetic control of grain quality traits in barley. Euphytica 2025, 221, 4. [Google Scholar] [CrossRef] [Scilit]
- Kumar, A.; Tun, T.T.; Kumar, V. Genome-wide identification and expression analysis of UDP-glycosyltransferases genes associated with secondary metabolism during grain development in pearl millet (Pennisetum glaucum). Plant Gene 2025, 44, 100541. [Google Scholar] [CrossRef] [Scilit]
- Rasheed, A.; Wen, W.; Gao, F.; Zhai, S.; Jin, H.; Liu, J.; Guo, Q.; Zhang, Y.; Dreisigacker, S.; Xia, X.; et al. Development and validation of KASP assays for genes underpinning key economic traits in bread wheat. Theor. Appl. Genet. 2016, 129, 1843–1860. [Google Scholar] [CrossRef] [Scilit]
- Tian, Y.; Liu, P.; Zhang, X.; Liu, Y.; Kong, D.; Nie, Y.; Xu, H.; Han, X.; Sang, W.; Li, W. Genome-wide association study and KASP marker development for starch quality traits in wheat. Plant Genome 2024, 17, e20514. [Google Scholar] [CrossRef] [Scilit]
- White, J.; Sharma, R.; Balding, D.; Cockram, J.; Mackay, I.J. Genome-wide association mapping of Hagberg falling number, protein content, test weight, and grain yield in UK wheat. Crop Sci. 2022, 62, 965–981. [Google Scholar] [CrossRef] [Scilit]
- Groos, C.; Robert, N.; Bervas, E.; Charmet, G. Genetic analysis of grain protein-content, grain yield and thousand-kernel weight in bread wheat. Theor. Appl. Genet. 2003, 106, 1032–1040. [Google Scholar] [CrossRef] [Scilit] [PubMed]


| GPC a (%) | WGC b (%) | |||||||
|---|---|---|---|---|---|---|---|---|
| 2022AY c | 2023AY | 2022YL | 2023YL | 2022AY | 2023AY | 2022YL | 2023YL | |
| Max | 18.4 | 18.4 | 18.1 | 18.1 | 13.8 | 14.0 | 13.7 | 13.8 |
| Min | 12.0 | 12.2 | 12.3 | 12.2 | 10.3 | 10.3 | 10.3 | 10.3 |
| Average | 14.7 | 14.7 | 14.7 | 14.7 | 11.9 | 11.9 | 11.9 | 11.9 |
| Standard deviation | 1.04 | 1.09 | 1.05 | 1.06 | 0.73 | 0.71 | 0.70 | 0.72 |
| Coefficient of variation | 0.070 | 0.074 | 0.071 | 0.070 | 0.062 | 0.060 | 0.059 | 0.060 |
| Name a | Environment | Chr. b | Position (Mb) | p-Value | R2 (%) |
|---|---|---|---|---|---|
| QGPC.zaas-1AS | E1, E2 | 1A | 32.3–32.3 | 2.8 × 10⁻⁴~3.0 × 10⁻⁴ | 8.2–8.4 |
| QGPC.zaas-3AL | E1, E2 | 3A | 725.3–732.1 | 6.6 × 10⁻⁴~6.8 × 10⁻⁴ | 7.3–7.4 |
| QGPC.zaas-3BL | E2, E2 | 3B | 751.8–751.8 | 8.3 × 10⁻⁴~8.3 × 10⁻⁴ | 7.1–7.8 |
| QGPC.zaas-4BL | E1, E2 | 4B | 650.0–650.0 | 5.1 × 10⁻⁴~5.7 × 10⁻⁴ | 6.0–6.1 |
| QWGC.zaas-4BL | E2, E2, E3 | 4B | 623.8–623.8 | 5.1 × 10⁻⁵~9.2 × 10⁻⁴ | 7.0–10.0 |
| QWGC.zaas-5A | E1, E2 | 5A | 446.0–446.0 | 5.5 × 10⁻⁴~5.7 × 10⁻⁴ | 7.4–7.6 |
| QWGC.zaas-5DS | E1, E3 | 5D | 34.6–34.6 | 4.7 × 10⁻⁴~5.0 × 10⁻⁴ | 7.6–7.7 |
| QTL a | Candidate | Chr. b | Position (Mb) | Annotation |
|---|---|---|---|---|
| QGPC.zaas-1AL | TraesCS1A01G049600 | 1A | 31.3 | ABC transporter family member |
| QGPC.zaas-3AL | TraesCS3A01G510200 | 3A | 730.3 | Abscisic stress ripening protein |
| QGPC.zaas-3AL | TraesCS3A01G512600 | 3A | 732.2 | Serine/threonine-protein kinase |
| QGPC.zaas-3BL | TraesCS3B01G506300 | 3B | 750.0 | F-box family protein |
| QWGC.zaas-4BL | TraesCS4B01G363300 | 4B | 652.2 | F-box family protein |
| QWGC.zaas-5A | TraesCS5A01G232300 | 5A | 447.5 | F-box family protein |
| QWGC.zaas-5DS | TraesCS5D01G034900 | 5D | 34.1 | UDP-glycosyltransferase |
| Kasp | QTL | Position (bp) | FAM | HEX | Common |
|---|---|---|---|---|---|
| Kasp-GPC-3AL | QGPC.zaas-3AL | 732,779,582 | cagttcaaagtgggatgttaaatgA | cagttcaaagtgggatgttaaatgG | ccttgatatgcatacatctggAaaT |
| Kasp-GPC-3BL | QGPC.zaas-3BL | 750,139,050 | TatcatagtagcaccacgcacgT | TatcatagtagcaccacgcacgC | atgaagcagagAggggaaTgaTaG |
| Kasp-GPC-4BL | QGPC.zaas-4BL | 649,605,374 | ttattttatcagcggCtgCatcgaT | ttattttatcagcggCtgCatcgaC | gAacatcccaaatgcgaaccaaC |
| Kasp-WGC-5AL | QWGC.zaas-5A | 444,264,937 | ggtgtatgacgcCgaattcA | ggtgtatgacgcCgaattcG | ggtGatAatttccttctcCgaatG |
| Kasp-WGC-5DS | QWGC.zaas-5DS | 31,273,513 | ctcatccatcaatgacatcatttcA | ctcatccatcaatgacatcatttcG | gcgacagtcttaccgaatcttc |
| Marker | QTL | Genotype | Number of Lines | Phenotype (%) | p Value |
|---|---|---|---|---|---|
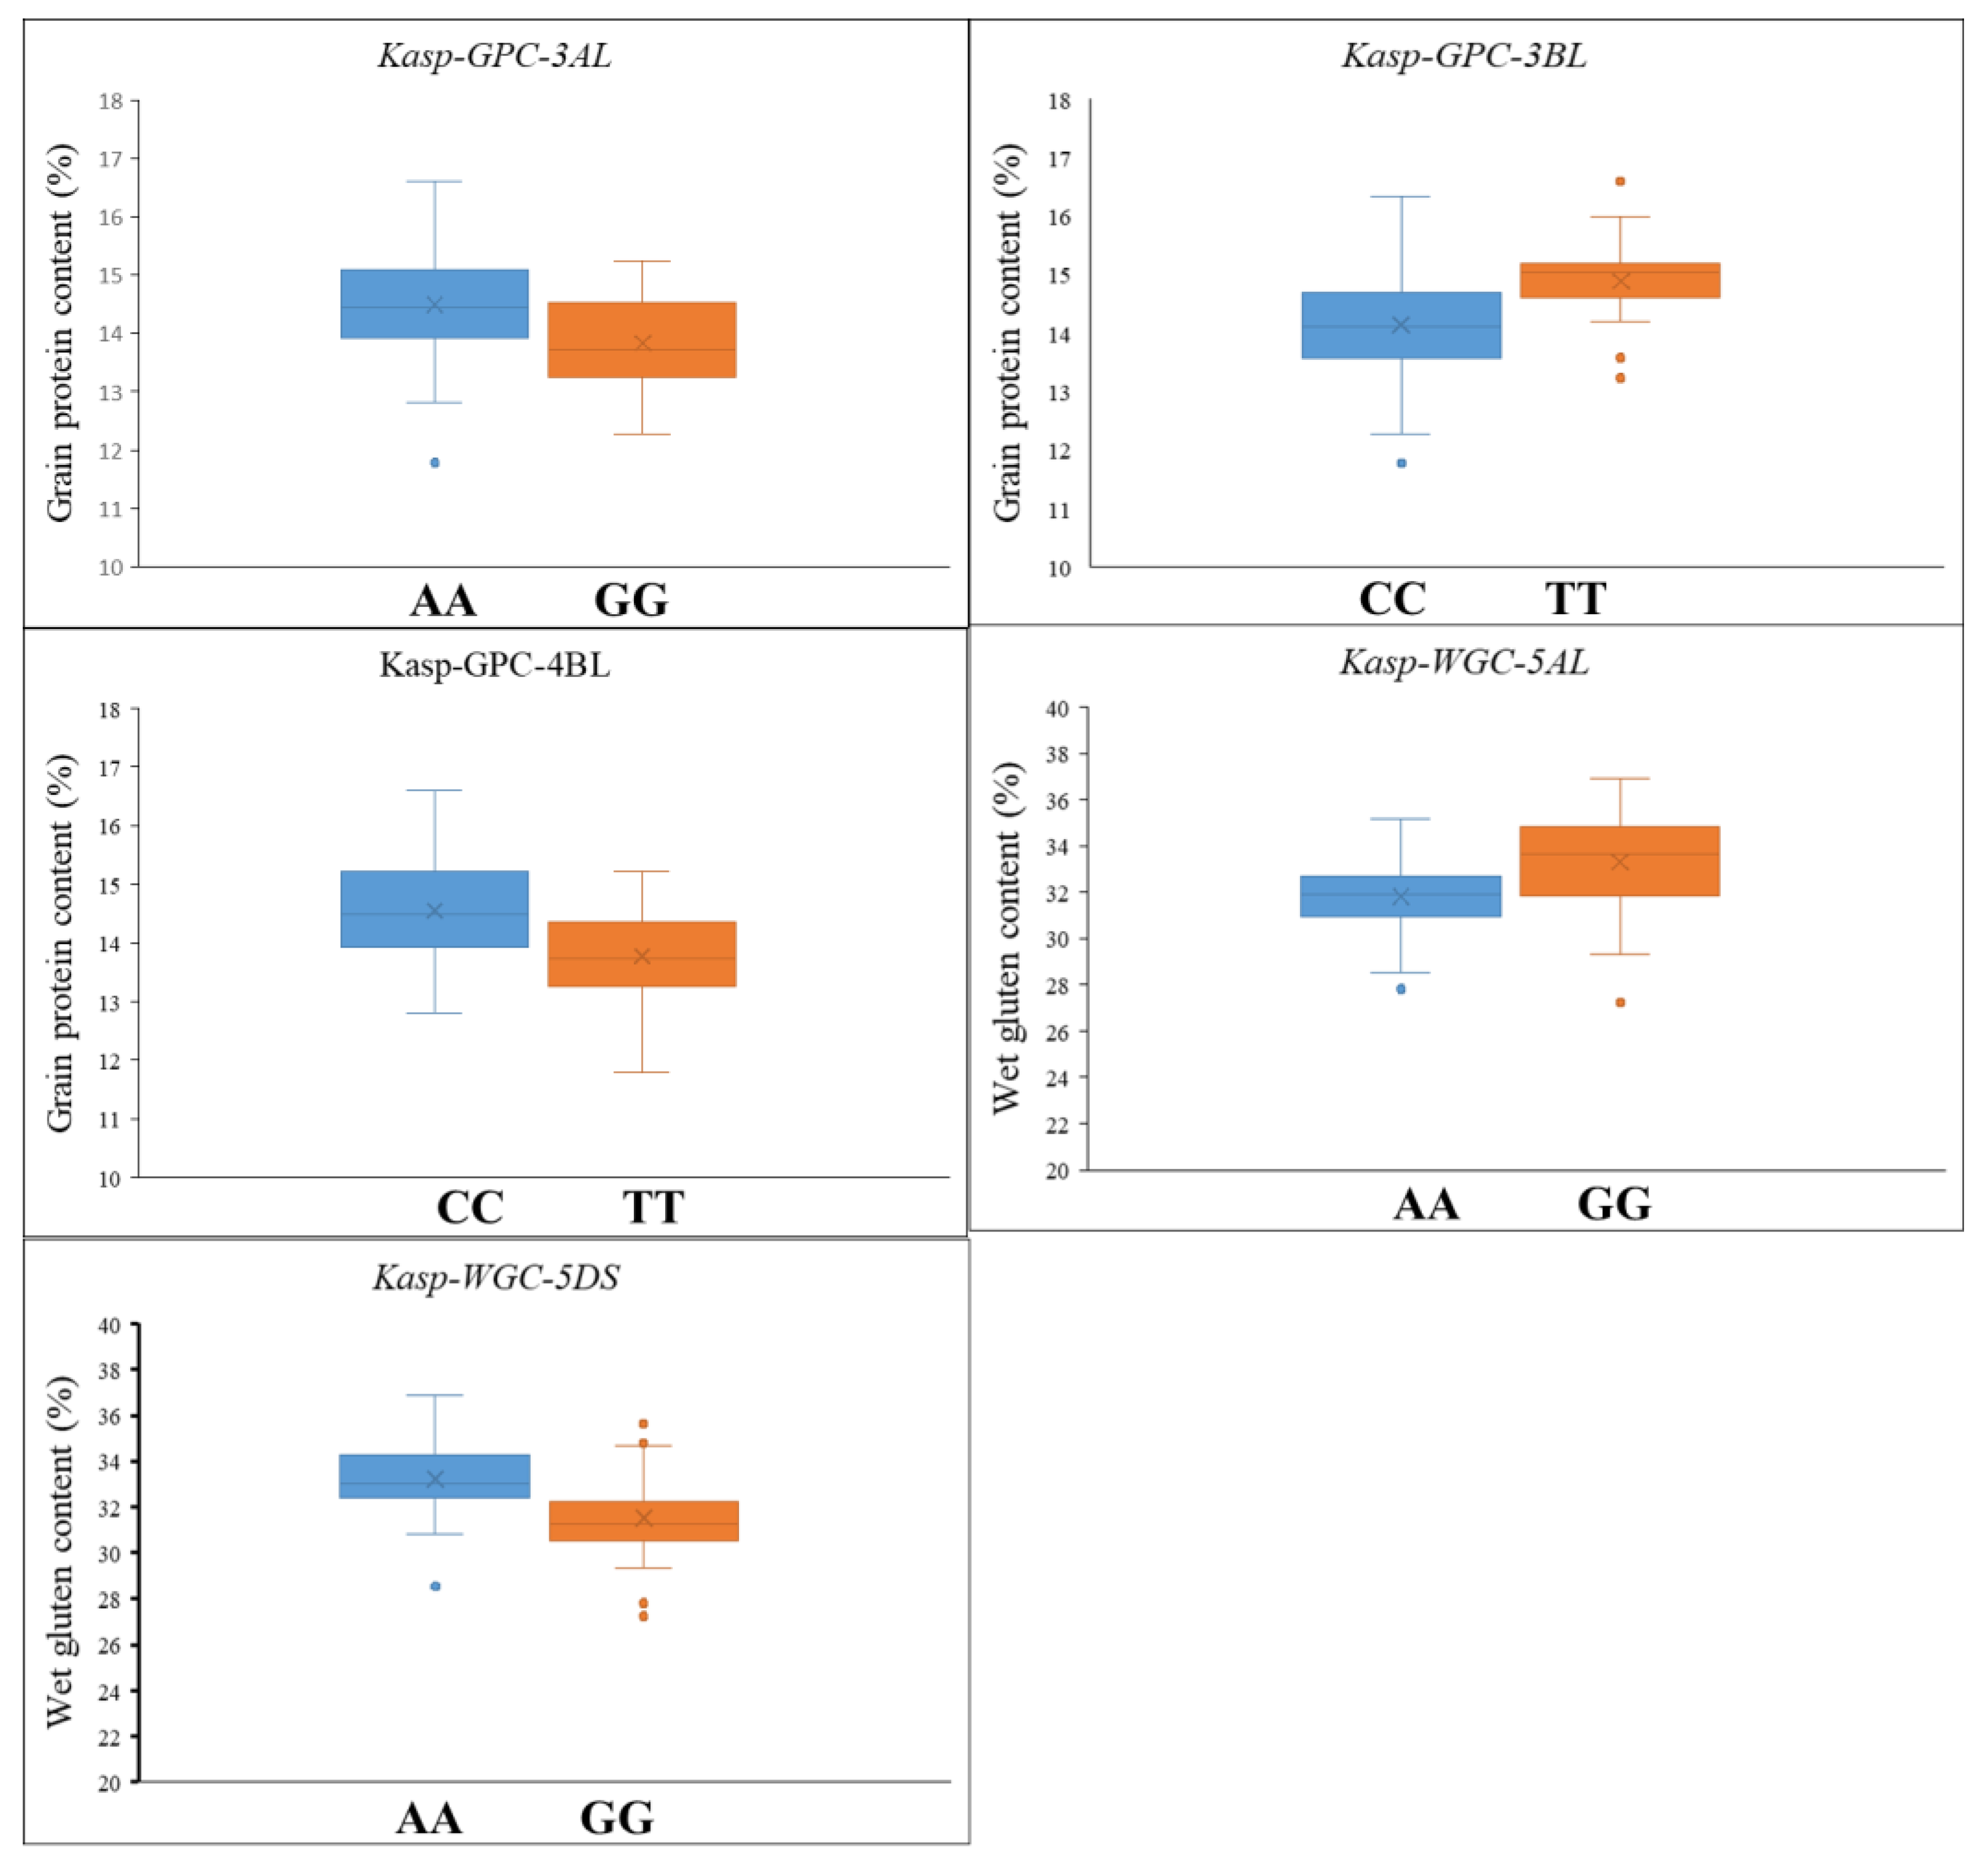
| Kasp-GPC-3AL | QGPC.zaas-3AL | AA | 84 | GPC: 14.5 | p < 0.01 |
| GG | 37 | GPC: 13.8 | |||
| Kasp-GPC-3BL | QGPC.zaas-3BL | TT | 23 | GPC: 14.9 | p < 0.01 |
| CC | 100 | GPC: 14.1 | |||
| Kasp-GPC-4BL | QGPC.zaas-4BL | TT | 31 | GPC: 13.8 | p < 0.01 |
| CC | 61 | GPC: 14.5 | |||
| Kasp-WGC-5A | QWGC.zaas-5A | AA | 82 | WGC: 31.8 | p < 0.01 |
| GG | 41 | WGC: 33.3 | |||
| Kasp-WGC-5DS | QWGC.zaas-5D | AA | 45 | WGC: 33.2 | p < 0.01 |
| GG | 47 | WGC: 31.5 |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.
Share and Cite
Song, Q.; Cui, W.; Gao, Z.; Song, J.; Wang, S.; Ma, H.; Chen, L.; Xu, K.; Jin, Y. Uncovering the Genetic Basis of Grain Protein Content and Wet Gluten Content in Common Wheat (Triticum aestivum L.). Plants 2026, 15, 307. https://doi.org/10.3390/plants15020307
Song Q, Cui W, Gao Z, Song J, Wang S, Ma H, Chen L, Xu K, Jin Y. Uncovering the Genetic Basis of Grain Protein Content and Wet Gluten Content in Common Wheat (Triticum aestivum L.). Plants. 2026; 15(2):307. https://doi.org/10.3390/plants15020307
Chicago/Turabian StyleSong, Quanhao, Wenwen Cui, Zhanning Gao, Jiajing Song, Shuaishuai Wang, Hongzhen Ma, Liang Chen, Kaijie Xu, and Yan Jin. 2026. "Uncovering the Genetic Basis of Grain Protein Content and Wet Gluten Content in Common Wheat (Triticum aestivum L.)" Plants 15, no. 2: 307. https://doi.org/10.3390/plants15020307
APA StyleSong, Q., Cui, W., Gao, Z., Song, J., Wang, S., Ma, H., Chen, L., Xu, K., & Jin, Y. (2026). Uncovering the Genetic Basis of Grain Protein Content and Wet Gluten Content in Common Wheat (Triticum aestivum L.). Plants, 15(2), 307. https://doi.org/10.3390/plants15020307