


Simple Summary
In recent years, blockages caused by marine organisms have increasingly threatened the cooling water systems of coastal nuclear power plants (NPPs). This study investigated the macrobenthic communities in three functional areas (water intake, harbor basin, and drainage outlet) adjacent to the Northeast Fujian NPP from 2018 to 2024. We analyzed community structure (species composition, biomass, density, and diversity) and its correlation with environmental factors. The results showed that the environmental factors affecting the changes in the macrobenthic community structure varied across different years in the waters adjacent to the Northeast Fujian NPP. Using the Grappler Method Risk Index, only two species (Protankyra bidentata (spiny sea cucumber) and Actiniaria sp. (sea anemone)) were identified as medium risks for blocking cooling water systems, while most other organisms were classified as low risk or extremely low risk. The Mantel test and random forest analysis revealed that nitrogen nutrients (NO3−) and phosphorus (PO43−) were significantly positively correlated with the polychaete community. Additionally, NO3− and NH4+ each explained 13.66% of the variation in the diversity index (H′), serving as key factors driving the macrobenthic community structure. This study provides scientific support for establishing a marine biological risk early-warning system and for the ecological security management of coastal NPPs.
Abstract
Cooling water systems of coastal nuclear power plants in China are frequently threatened by blockages caused by marine organisms. However, long-term studies on macrobenthic community dynamics and their associations with environmental factors are scarce, limiting the precise prevention of such blockage risks. This study conducted quantitative monitoring of macrobenthos and synchronous measurement of water environmental factors at 24 sampling stations in three functional areas (water intake, harbor basin, and drainage outlet) adjacent to the Northeast Fujian NPP from 2018 to 2024. Community structure characteristics were analyzed using the Shannon–Wiener and Margalef indices. The Grappler Method Risk Index (GMRI) was employed to screen species at risk of blocking cooling water systems, and the Mantel test and random forest models were applied to explore the associations between the macrobenthic community and environmental factors. A total of 161 macrobenthic species were identified. Polychaetes (71 species, accounting for 44.1%) were the absolute dominant group, followed by crustaceans (35 species) and Mollusks (30 species). The interannual fluctuation range of the polychaete proportion was 41.1–57.8%, reaching a peak in 2023. There were significant differences in community structure among different areas (PERMANOVA, p < 0.05), with the largest inter-regional difference in 2024 (R2 = 0.36). The annual average number of species (9 species), density (155.25 ind./m2), and biomass (29.58 g/m2) in the drainage outlet were higher than those in the water intake and harbor basin. The GMRI identified Protankyra bidentata (spiny sea cucumber, GMRI values of 50.67% to 64.98% from 2019 to 2023) and Actiniaria sp. (sea anemone, a GMRI value of 54.63% in 2021) as medium-risk species for cooling water system blockage, while most other organisms were classified as low risk or extremely low risk. The Mantel test and random forest analysis confirmed that nitrogen nutrients (NO3−) and phosphorus (PO43−) were significantly positively correlated with the polychaete community. Furthermore, NO3− and NH4+ each explained 13.66% of the variation in the diversity index (H′), serving as key factors driving community structure. This study demonstrates the co-dominance of thermal and nutrient drivers in shaping macrobenthic communities over a multi-year scale, and identifies specific, morphologically suited taxa as potential blockage risks. The findings provide a scientific basis for targeted risk-species monitoring and support the integration of long-term ecological data into NPP cooling water system security management.
1. Introduction
The abnormal aggregation (e.g., outbreaks and biofouling) of marine organisms poses a significant threat to the safety of water intake in cooling water systems in coastal nuclear power plants (NPPs) [1,2,3]. Over the past few decades, such phenomena have compromised the safety of cooling water systems in coastal nuclear power plants worldwide [4,5,6,7]. For instance, in December 2009, Unit 4 of France’s CRUAS Nuclear Power Plant experienced a cooling source failure due to waterweed blockage [8]. Swedish nuclear power plants were forced to shut down following jellyfish outbreaks [9]. South Korea’s Uljin Nuclear Power Plant experienced a 38% drop in power generation capacity due to blockage by Salpa fusiformis [10]. In China, similar challenges have been reported, such as the shutdown of the Hongyanhe NPP following an Aurelia aurita bloom [11] and reduced filter efficiency at the Ningde NPP due to Acaudina molpadioides [12,13]. Such incidents have resulted in economic losses totaling billions of US dollars [2,14]. According to statistics, among nearly 200 nuclear power plant water intake blockage incidents globally, 84% were triggered by marine organisms [4,15]. Therefore, systematic research on the mechanisms behind marine organism-induced blockages is urgently needed to inform effective prevention strategies.
Previous studies have mainly focused on marine organism outbreaks [3,4,16,17], acoustic imaging and numerical simulation [16,18,19,20], optimization of water intake design [21,22], accumulation of marine debris [23], and early warning and prevention/control methods [2]. Meanwhile, monitoring and early warning systems, as well as decision support systems targeting marine organisms in NPP cooling water systems, have been developed and put into use [8,24,25,26,27,28,29]. Some scholars have predicted biomass in waters adjacent to NPPs by establishing models [30,31], identifying the area within 1 km of the cooling source as a high-risk zone. Others have attempted to integrate acoustic imaging with numerical simulation, using multi-beam sonar [16] or the FVCOM model [32] to predict the migration pathways of risk-associated organisms.
However, existing research on marine organism-induced blockage risks in NPP cooling water systems still has shortcomings. Wu et al. (2023) [17] found that the abundance of spring zooplankton in Daya Bay reached as high as 1372.01 ind./m3, and aggregation of gelatinous organisms (Dolioletta gegenbauri) is prone to causing blockages; however, their study was based only on one year of survey data. He et al. [33] and Wang Yu et al. [7] screened multiple high-risk phytoplankton species that tend to form communities or aggregations by combining one year of survey data with historical data. Hu et al. [34] analyzed the thermal discharge effects of China’s Daya Bay NPP and found that a 5–10 °C increase in surface water temperature significantly alters phytoplankton community composition, though this finding was based on a single survey and limits its reflection of temporal dynamics. Huang et al. (2025) [5] conducted an annual survey of nekton in waters adjacent to Northeast Fujian NPP, indicating that the risk of nekton induced cooling water blockage is highest between May and October. Lou et al. (2023) [35] simulated the movement of krill using 250,000 passive particles and found that Acetes chinensis forms “path-dependent aggregation” through the Lagrangian Flow Network (LFN) after 30 days of tracking. Most of the aforementioned studies are based on short-term survey data (one year or less), making it difficult to reflect the long-term dynamics of the macrobenthic community structure. Simultaneously, research on the correlations between macrobenthic communities and environmental factors remains insufficient.
Although Northeast Fujian NPP has conducted research on macrobenthos [12,13,36,37], jellyfish [38,39], plankton [40,41], and nekton [5,42], a comprehensive understanding of long term time series monitoring of macrobenthos is still lacking, especially the changing trends of the biological community structure on a nearly 5-year time scale and their long-term response mechanisms to environmental factors. Therefore, based on nearly 5 years of survey data (2018–2024) from the benthos of the water intake, harbor basin, and drainage outlet of Northeast Fujian NPP, this study analyzes the interannual changes in species composition, density, biomass, diversity indices, and dominant species of macrobenthos in this area. It also screens and evaluates macrobenthos species that may block the cooling water system, identifies potential risk-associated species, and explores the correlations between community structure and environmental factors. This research provides scientific data to support early warnings of macrobenthos risk, ecological security management, and cooling water system protection of coastal NPP projects.
2. Materials and Methods
2.1. Sample Stations
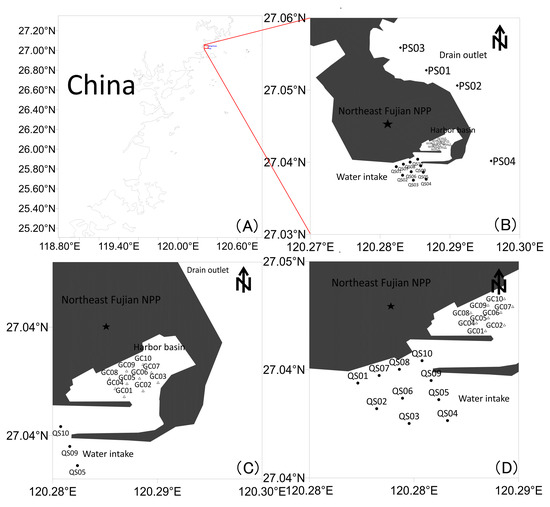
This study was conducted in the waters adjacent to the Northeast Fujian Nuclear Power Plant (NPP), Fujian, China (27.03° N–27.06° N, 120.27° E–120.30° E). The data used in this study were derived from the quantitative monitoring of macrobenthos carried out by Ningde Marine Center in the study area from 2018 to 2024. Sampling was not conducted in 2022 due to safety concerns from frequent typhoons. A total of 24 sampling stations were deployed, with sampling conducted annually in either July or October. Based on the hydrological characteristics of the NPP-adjacent waters, the monitored area was divided into three functional zones, including water intake (QS01–QS10), drainage outlet (PS01–PS04), and harbor basin (GC01–GC10), with 10, 4, and 10 sampling stations, respectively (Figure 1).
Figure 1.
Map of sampling stations adjacent to the Northeast Fujian Nuclear Power Plant. (A) Geographic overview map. (B) Detailed map of the drain outlet zone (PS01–PS04). (C) Detailed map of the harbor basin zone (GC01–GC10). (D) Detailed map of the water intake zone (QS01–QS10). Star represents the location of Northeast Fujian Nuclear Power Plant.
2.2. Macrobenthos Collection and Analysis
Biological samples were collected in accordance with the protocols specified in the Marine Monitoring Specifications [43]. A 0.1 m2 grab sampler was employed, and two replicates were collected at each station and combined into one quantitative sample. Sediment samples were rinsed through a sieve with an aperture of 0.5 mm to retain macrobenthos. Biomass was weighed using an electronic balance with a precision of 0.001 g (Model WT3003, Serial Number 1999). The taxonomy of macrobenthic species followed the World Register of Marine Species (WoRMS) database [44] (http://www.marinespecies.org, accessed on 25 April 2025) and was cross-verified against Checklist of Marine Biota of China Seas [45].
2.3. Environmental Factor Measurement
Concurrent with biological sampling, key water quality parameters were monitored at each station following the national standard Marine Monitoring Specifications—Part 4: Seawater Analysis (GB 17378.4-2007) [46]. Water quality parameters included temperature (WT, °C), salinity (SAL), pH, dissolved oxygen (DO, mg/L), chemical oxygen demand (COD, mg/L), reactive phosphate (PO43−, mg/L), nitrite (NO2−, mg/L), nitrate (NO3−, mg/L), ammonium (NH4+, mg/L), and suspended solids (SS, mg/L).
2.4. Data Analysis
The interannual changes in the community structure of macrobenthos in the waters adjacent to Northeast Fujian NPP were analyzed using the Shannon–Wiener index (H′) [47], Margalef’s richness index (d) [48], and Pielou’s evenness index (J′) [49], with calculation methods referring to the cited studies.
Dominance () was used to identify dominant species at each station. A species was considered dominant when > 0.02 [50], calculated as follows:
where = the frequency of occurrence of the i-th species across all sampling stations.
The risk of macrobenthos causing cooling water system blockage was evaluated using the Grappler Method Risk Index (GMRI) [12], which was developed by Cai et al. (2022) specifically for assessing the risk of benthic macrofauna entrapment in coastal nuclear power plant cooling water systems.
GMRI = (A + B + P + F + C) × 20%
A (percentage of abundance) = the percentage of the average density of the target species relative to the average density of all macrobenthos.
B (percentage of biomass) = the percentage of the average biomass of the target species relative to the average biomass of all macrobenthos; P (percentage of sampling stations) = the frequency of occurrence of the target species across all stations; F (floating risk) = the potential of the species to float with water flow; and C (water-flow-driven risk) = the potential of the species to be transported by water flow to the cooling water intake.
Risk classification based on GMRI values: GMRI ≥ 90%, extremely high risk; 70% ≤ GMRI < 90%, high risk; 50% ≤ GMRI < 70%, medium risk; 30% ≤ GMRI < 50%, low risk; and GMRI <30%, extremely low risk.
2.5. Statistical Analysis
SPSS 27 software was used to perform one-way Analysis of Variance (ANOVA) on environmental factors, with the water intake, harbor basin, and drainage outlet as fixed factors. Prior to analysis, the Shapiro–Wilk test was used to verify data normality, and the Levene test was used to check homogeneity of variances. Water quality environmental factors were subjected to logarithmic transformation (log10(raw data + 1)) to meet the requirements of normality and homogeneity of variances. For data with homogeneous variances, Tukey’s HSD test was used for post hoc multiple comparisons.
R software (version 4.10) was used for subsequent analyses. Species abundance data were subjected to a square root transformation, and Principal Coordinates Analysis (PCoA) was constructed based on the Bray–Curtis similarity matrix. Permutational Multivariate Analysis of Variance (PERMANOVA) with 999 permutations was used to test inter-group differences.
The Mantel test (linkET package version 0.0.7.4) was performed to analyze the correlation between macrobenthic community structure and environmental factors.
Random forest analysis (randomForest package version 4.7.1.1) was conducted with the diversity index (H′) as the response variable and environmental factors as explanatory variables. Factor importance was calculated using node impurity (Gini coefficient) with 1000 permutations.
Graphs of species composition and diversity trends were plotted using Prism 10.0. One-way ANOVA combined with Tukey’s post hoc test was used to compare differences in biological indices across different areas, with the significance level set at p < 0.05. The sampling station map was prepared using Surfer 16 software (https://www.goldensoftware.com/products/surfer/ (accessed on 25 November 2025)).
3. Results
3.1. Species Composition of Macrobenthos
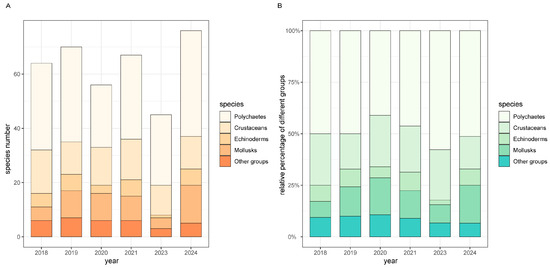
From 2018 to 2024, quantitative monitoring samples from the waters adjacent to Northeast Fujian NPP were analyzed, resulting in the identification of 161 macrobenthic species, among which 12 were identified at the genus level. Polychaetes were the most abundant group, with 71 species accounting for 44.1% of the total, followed by crustaceans (35 species, 21.7%), Mollusks (30 species, 18.6%), and Echinoderms (10 species, 6.2%). Other groups included Chordates, Cnidarians, Latyhelminths, Nemerteans, Sipunculans, and Echiurans (Table 1, Figure 2).
Table 1.
Composition of macrobenthic species from 2018 to 2024.
Figure 2.
Interannual variation in number of species of macrobenthic taxa from 2018 to 2024. (A) Total species number of different macrobenthic taxa. (B) Relative percentage of different macrobenthic taxa.
Polychaetes remained the dominant group, accounting for 50.0% of the total species in 2018 and 2019, decreasing to 41.1% in 2020, and then recovering to 46.3% in 2021 and 51.3% in 2024, with a peak of 57.8% in 2023 (with an interannual fluctuation range from 41.1% to 57.8%). Crustaceans, the second-largest group, decreased year by year from 25.0% in 2018 to 15.8% in 2024, with a slight recovery to 25.0% in 2020 (interannual fluctuation range from 15.8% to 25.0%). Mollusks, the third-largest group, increased significantly to 14.3% in 2019 and 17.9% in 2020, dropped to 8.9% in 2023, and rose again to 18.4% in 2024 (interannual fluctuation range from 7.8% to 18.4%). Echinoderms, the fourth-largest group, accounted for 8.6% in 2019, decreased to 5.4% in 2020, recovered to 9.0% in 2021, fell to 2.2% in 2023, and rebounded to 7.9% in 2024. In most years, only one species was recorded in other groups (Cnidarians, Platyhelminths, Nemerteans, Sipunculans, and Echiurans).
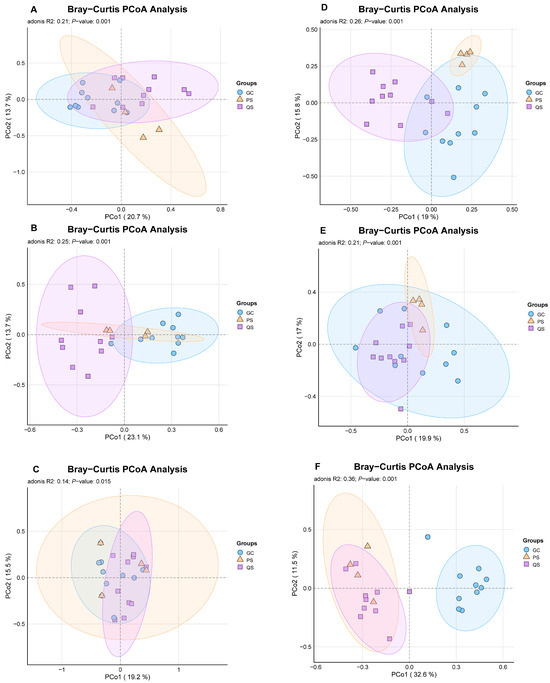
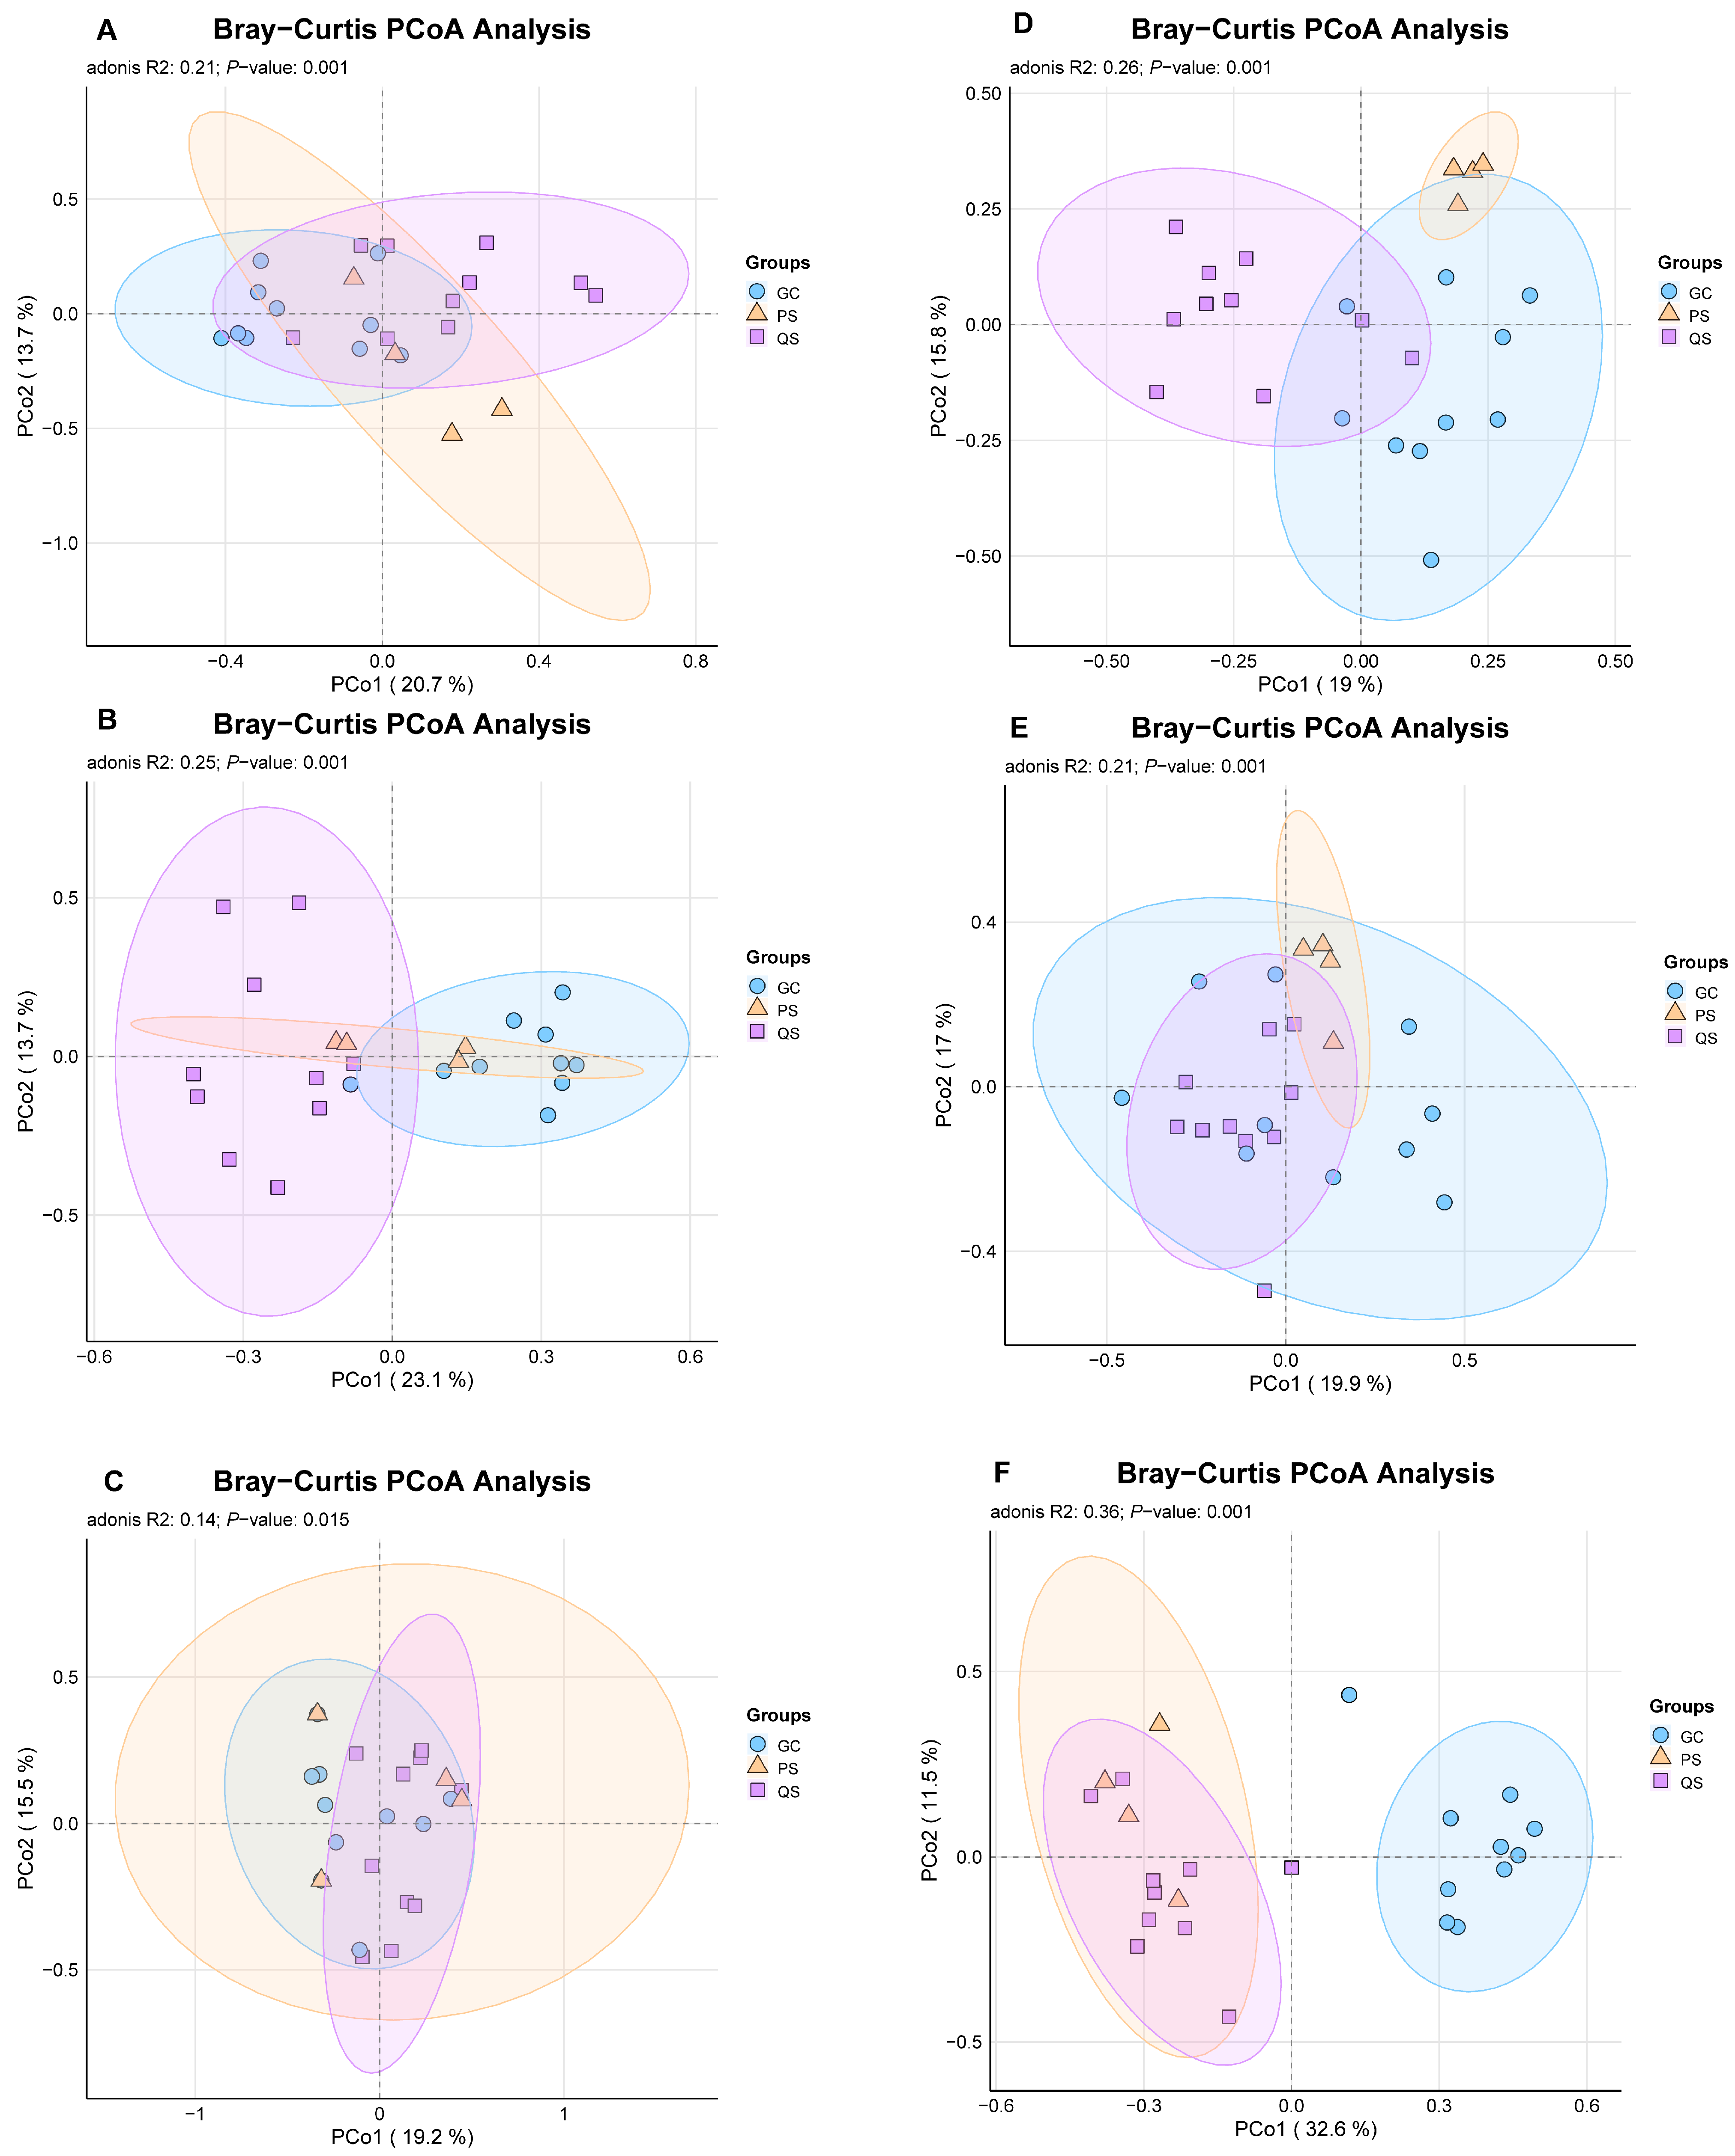
The results of Principal Coordinates Analysis (PCoA) and Permutational Multivariate Analysis of Variance (PERMANOVA) (Figure 3) showed significant differences in macrobenthic communities among different areas. In 2018, PC1 accounted for 20.7% of the total variance with clear significant differences among groups (Figure 3A). In 2019, PC1 accounted for 23.1%, reflecting more pronounced inter-group differences than those observed in 2018 (Figure 3B). In 2020, although statistical significance was slightly attenuated, distinct differences still persisted among groups with PC1 and PC2, explaining 19.2% and 15.5% of the variance, respectively (Figure 3C). The year 2021 saw PC1 contributing 19% and PC2 contributing 15.8% of the total variance (Figure 3D). In 2023, PC1 and PC2 accounted for 19.9% and 17% of the variance, respectively, with significant inter-group differences remaining evident (Figure 3E). Notably, 2024 showed the most striking pattern across all study years as PC1 alone explained 32.6% of the variance, indicating that inter-group differences were particularly prominent along the PC1 axis and sample separation was consequently more distinct (Figure 3F). Overall, there were significant differences in macrobenthic community structure among groups in each year, with the highest inter-group difference in 2024 and the relatively lowest in 2020.
Figure 3.
PCoA plots of macrobenthic communities with PERMANOVA test from 2018 to 2024. Different colors represent functional zones: purple = water intake (QS); blue = harbor basin (GC); yellow = drainage outlet (PS). (A) 2018 PCoA analysis of macrobenthic communities; (B) 2019 PCoA analysis of macrobenthic communities; (C) 2020 PCoA analysis of macrobenthic communities; (D) 2021 PCoA analysis of macrobenthic communities; (E) 2023 PCoA analysis of macrobenthic communities; (F) 2024 PCoA analysis of macrobenthic communities.
3.2. Number of Species, Biomass, Density, and Diversity Indices of Macrobenthos
From 2018 to 2024, the annual number of macrobenthic species in the study area ranged from 45 to 76, with an annual average of 63. The total number of species showed a fluctuating upward trend, reaching the highest point in 2024 (an increase of approximately 20% compared to 2018). At the group level, the number of species in major groups such as polychaetes and crustaceans also showed a fluctuating upward trend, while those of Mollusks and Echinoderms remained relatively stable, and the number of species in other groups exhibited a slight downward trend.
In terms of spatial distribution, the number of species in the water intake (QS), harbor basin (GC), and drainage outlet (PS) was generally low and showed a fluctuating pattern. One-way ANOVA revealed no significant differences in the number of macrobenthic species across the three areas in 2019, 2020, 2021, and 2023 (p > 0.05), while significant differences were observed in 2018 (F2 = 5.14, p < 0.05), and highly significant differences were observed in 2024 (F2 = 11.62, p < 0.01).
From 2018 to 2024, the annual average density of macrobenthos in the study area ranged from 38.26 ind./m2 to 220.29 ind./m2, with an annual mean of 97.33 ind./m2, reaching the highest in 2024 and the lowest in 2020. The annual biomass ranged from 7.76 g/m2 to 24.01 g/m2, with an annual mean of 16.98 g/m2, peaking in 2020 and bottoming out in 2023.
Spatial differences were observed among the three areas with the drainage outlet (PS) exhibiting the highest annual average number of species (9), density (155.25 ind./m2) and biomass (29.58 g/m2) in comparison to the harbor basin (GC) which had 7.3 species, density (80.86 ind./m2) and biomass (15.09 g/m2) and the water intake (QS) which had nine species, density (110.50 ind./m2) and biomass (14.49 g/m2). Across all sampling years, the drainage outlet (PS) recorded the highest number of species density and biomass in 2024.
One-way ANOVA showed no significant differences in macrobenthic density among the three areas in 2019, 2020, 2021, and 2024 (p > 0.05), but significant differences were detected in 2018 (F2 = 6.01, p < 0.01) and 2023 (F2 = 4.466, p < 0.05). For biomass, no significant differences were found among the three areas in 2018, 2019, 2021, 2023, and 2024 (p > 0.05), while highly significant differences were observed in 2020 (F2 = 6.713, p < 0.01).
The macrobenthic community diversity index (H′) in the waters adjacent to Northeast Fujian NPP ranged from 2.15 to 2.93, with an annual average of 2.57, reaching the highest value in 2024. The richness index (d) ranged from 0.80 to 1.28 (annual average value 1.09), and the evenness index (J′) ranged from 0.79 to 0.94 (annual average value 0.90).
No significant differences were found in the diversity index (H′) among areas in 2019, 2020, 2021, and 2023 (p > 0.05), but significant differences were observed in 2018 (F2 = 4.30, p < 0.05) and highly significant differences were identified in 2024 (F2 = 16.11, p < 0.01). No significant differences in the richness index (d) were detected among areas in 2019, 2020, 2021, and 2023 (p > 0.05), while significant differences were found in 2018 (F2 = 4.25, p < 0.05) and highly significant differences in 2024 (F2 = 18.12, p < 0.01). No significant differences in the evenness index (J′) were observed among areas in 2018, 2019, 2020, 2021, and 2024 (p > 0.05), but significant differences were found in 2023 (F2 = 5.48, p < 0.05).
Overall, no obvious consistent differences were observed in the diversity, richness, and evenness indices among the water intake, harbor basin, and drainage outlet. Comprehensively considering the three indices, the biodiversity in the drainage outlet was lower than that in other areas in most years.
3.3. Dominant Species, GMRI, and Their Correlations with Environmental Factors
The dominant species of macrobenthos and their corresponding dominance values in the waters adjacent to the NPP during the period 2018–2024 (Table 2). During this period, the primary dominant species were Notomastus cf. aberans, Protankyra bidentata, and Heteromastus filiformis. In 2018, the dominant species at the water intake (QS) was Gammaridean sp. with a dominance value of 0.148, while the dominant species at the harbor basin (GC) was Notomastus cf. aberans (0.072) and that at the drainage outlet (PS) was Notomastus cf. aberans (0.079). In 2019, the dominant species at QS was Xantho distinguendus (0.097), while that at GC was Protankyra bidentata (0.185) and that at PS was Notomastus cf. aberans (0.125). In 2020, the dominant species at QS was Aglaophamus dibranchis (0.066), while that at GC was Nassarius semiplicatus (0.045) and that at PS was Notomastus cf. aberans (0.129). In 2021, the dominant species at QS was Actiniaria sp. (0.190), whereas that at GC was Protankyra bidentata (0.430) and that at PS was Paraprionospio sp. (0.040). In 2023, Heteromastus filiformis was the dominant species at both QS (0.165) and PS (0.667), while that at GC was Notomastus cf. aberans (0.151). In 2024, the dominant species at QS was Gammaridean sp. (0.355), whereas that at GC was Polydora sp. (0.694) and that at PS was Sternaspis scutata (0.082). Among these dominant taxa, polychaetes were predominantly represented by Notomastus cf. aberans, Echinoderms were represented by Protankyra bidentata, and crustaceans were represented by Xantho distinguendus and Gammaridean sp. A total of 19 dominant species were recorded at QS, with Xantho distinguendus, Glycera chirori, and Gammaridean sp. occurring in more than two years.
Table 2.
Dominant species of macrofauna in the adjacent sea area of Northeast Fujian Nuclear Power Plant (dominant species/dominance value).
At GC, 23 dominant species were identified, with Notomastus cf. aberans and Protankyra bidentata species occurring in more than two years, and Notomastus cf. aberans species appearing continuously dominant in 2018, 2021, and 2023. At PS, 15 dominant species were documented, with Notomastus cf. aberans persistently dominant from 2018 to 2023. Overall, Notomastus cf. aberans and Protankyra bidentata were distributed as dominant species across all three areas, with Heteromastus filiformis also found to be a common dominant taxon. Protankyra bidentata predominantly inhabits muddy substrates of coastal shallow seas and is widely distributed from the Bohai Sea to the Beibu Gulf of China; it is a prevalent species in nearshore ecosystems. Actiniaria sp. prefers hard substrates near water intakes, where it attaches to rocks or artificial structures and secretes viscous substances. Other dominant species, such as Notomastus cf. aberans and Heteromastus filiformis, are typical detritivores adapted to high-nutrient sediment environments.
Based on the density, biomass, and collection frequency of macrobenthos obtained in the waters adjacent to Northeast Fujian NPP from 2018 to 2024, the GMRI was calculated for 11, 12, 10, 15, 10, and 13 macrobenthic species in each respective year (Table 3). The results indicated that Protankyra bidentata (spiny sea cucumber) and Actiniaria sp. (sea anemone) posed a medium risk of blocking the NPP’s cooling water system, while most other organisms were classified as low risk, and some others as extremely low risk.
Table 3.
Potential risk levels of macrobenthos blocking the cooling water system of Northeast Fujian NPP in adjacent waters (2018–2024).
The highest GMRI value (64.98%) was recorded for Protankyra bidentata in 2019, and the lowest (18.62%) value was recorded for Trigonothracia jinxingae in 2024. For Protankyra bidentata, the GMRI values reached 64.98% (July 2019), 50.67% (October 2020), 60.80% (July 2021), and 52.51% (October 2023), all falling into the medium-risk category. Additionally, its biomass proportion ranged from 11.75% to 53.66% during these periods. The GMRI of Actiniaria sp. only reached 54.63% (medium risk) in July 2021.
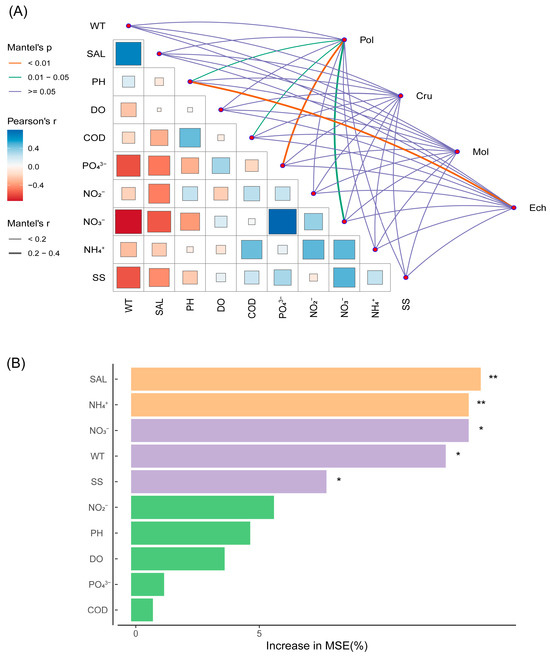
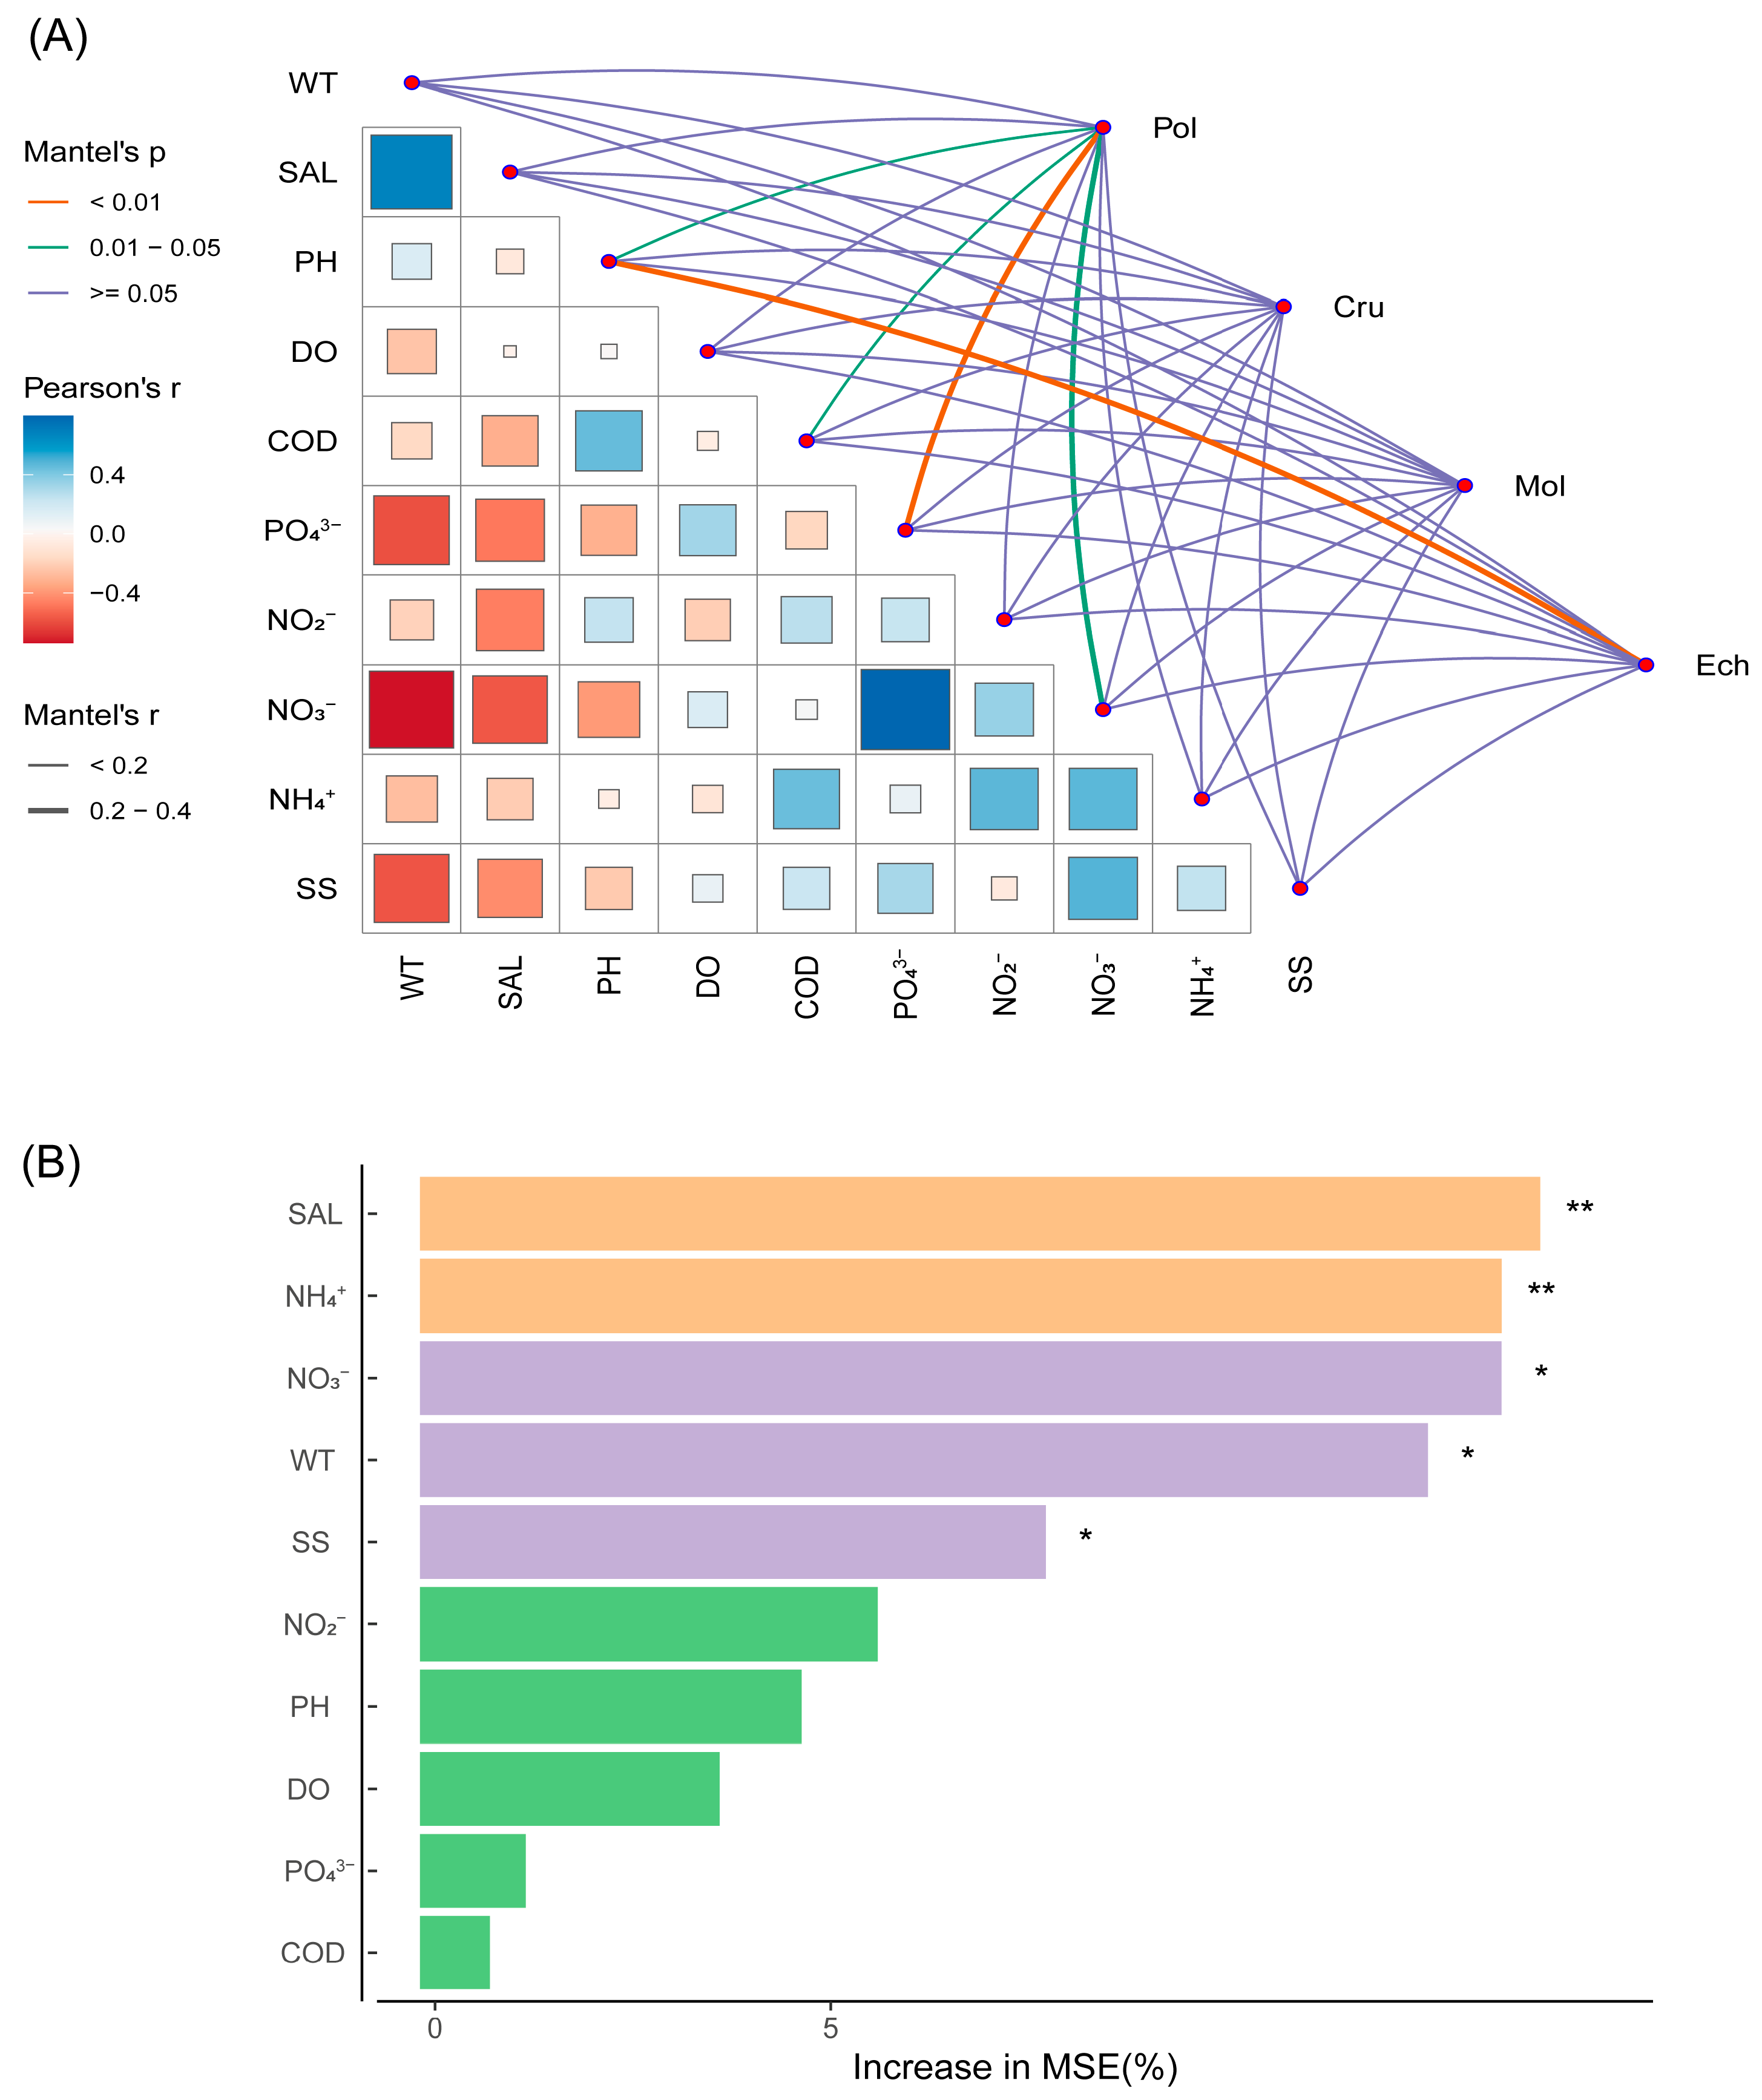
The results of the Mantel test analysis between subtidal macrobenthic communities and environmental factors from 2018 to 2024 showed that waterborne PO43− had a highly significant effect on the polychaete community (p < 0.01), and the community was also significantly affected by pH, COD, and NO3− (p < 0.05). For the echinoderm community, water pH exerted a highly significant effect (p < 0.01) (Figure 4A).
Figure 4.
(A) Macrobenthic Mantel analysis; (B) key environmental factors affecting H′ identified by random forest analysis. * indicates significant importance at p < 0.05, and ** indicates highly significant importance at p < 0.01.
Random forest analysis of the correlation between the macrobenthic diversity index (H′) and environmental parameters indicated that the key water quality factors influencing H′ were SAL (Salinity), NH4+, NO3−, WT (water temperature), and SS (suspended solids). These factors explained 14.14%, 13.66%, 13.66%, 12.73%, and 7.90% of the variation in H′, respectively (Figure 4B).
4. Discussion
4.1. Spatio-Temporal Dynamics of the Macrobenthic Communities
The results of this study revealed significant interannual variation and spatial differences in the macrobenthic community structure adjacent to Northeast Fujian NPP. Throughout the monitoring period, polychaetes remained the dominant taxonomic group. This persistent dominance is closely linked to their high physiological tolerance to environmental perturbations. Most polychaetes possess euryhaline and eurythermal traits [51], enabling them to withstand moderate thermal fluctuations and salinity variations associated with coastal runoff and NPP thermal discharge. Their capacity for cutaneous respiration also permits survival in episodically hypoxic conditions, particularly near the drain outlet (PS), where organic matter accumulates.
Thermal discharge from the Northeast Fujian NPP increases local seawater temperatures by 2.0–3.0 °C relative to the intake (QS) and harbor basin (GC) areas (Table 4). This warming likely accelerates organic matter decomposition in the water column and sediments [52], increasing the availability of detrital resources for deposit-feeding polychaetes. The enhanced food supply probably supports their numerical dominance and sustained population growth over the years. Spatially, biomass and density were consistently highest in the PS zone across most years. This pattern aligns with the thermal enhancement of metabolic rates and organic matter turnover, which collectively create a more favorable habitat for polychaetes [23,53] and is consistent with previous studies reporting elevated macrobenthic abundance near thermal discharge plumes [54,55]. Thermal input may also weaken water column stratification, promote nutrient upwelling, and modify microhabitat conditions in ways that further facilitate macrobenthic growth [23].
Table 4.
Water temperature at water intake, drain outlet and harbor basin from 2018 to 2024.
However, one-way ANOVA indicated no statistically significant spatial differences in univariate community metrics among the three zones in most years. This suggests that the operational impacts of the NPP remain within the coastal ecosystem’s current capacity for self-regulation. Nevertheless, the long-term cumulative effects of thermal discharge and nutrient enrichment on community structure warrant continued monitoring, as subtle shifts in species composition and functional traits may emerge over time.
In contrast to polychaetes, the relative abundance of crustaceans displayed a clear declining trend. This decrease is likely associated with sediment hypoxia driven by eutrophication, which can impair the respiratory physiology of crustaceans—a group generally sensitive to low dissolved oxygen (DO) levels. The PS area, in particular, is prone to seasonal DO depletion due to high organic loading, which may suppress reproduction, survival, and recruitment success.
This study recorded 161 macrobenthic species in the NPP-adjacent waters, with an average abundance of 97.33 ind./m2 and an average biomass of 16.98 g/m2. These values are higher than those reported from other coastal power plant areas in Fujian and Guangdong by Cai Lizhe et al. [12], Lin Xiuchun et al. [56], and Zhang et al. [40], but lower than the higher diversity documented at the Sanmen NPP (Zhou et al. [57,58]), and the Gori NPP in Korea (Yu et al. [59]) (Table 5). The higher species number, abundance, and biomass observed in this study compared to previous surveys and adjacent sea studies may be attributed to three reasons: The 6-year survey period covered interannual cycles of macrobenthic communities, such as reproduction and migration. As emphasized by Hines and Pereira et al. [60], Magurran [61], and Menger [62], long-term monitoring data help reveal the true state of biodiversity. The higher species number compared to previous studies [12,56,63] may be related to the enhanced adaptability of heat-tolerant species induced by thermal discharge [53]. The sampling stations in this study covered areas such as the harbor basin, water intake, and drainage outlet, providing more comprehensive coverage than previous studies [12,40,56] and thus better reflecting the macrobenthic community diversity in the NPP-adjacent waters [64].
Table 5.
Species richness, abundance, and biomass of macrobenthic communities in adjacent waters of different nuclear power plants.
4.2. Potential Risk of Macrobenthos to Cooling Water System Blockage
The observed ecological shifts in the macrobenthic community have direct implications for the operational security of the Northeast Fujian NPP, specifically the risk of blockage in the cooling water system. Using the GMRI, we identified two medium-risk species for Northeast Fujian NPP cooling water blockage: Protankyra bidentata (spiny sea cucumber) and Actiniaria sp. (sea anemone). The blockage risk associated with these organisms stems from their unique morphological and behavioral traits [12,56], which determine their potential to reach and accumulate on cooling water intake screens.
Protankyra bidentata exhibited a persistent medium risk (GMRI 50.67–64.98%) from 2019 to 2023. This species is common in the subtidal zones of bays such as Xinghua Bay [56,65], Dayawan Bay [66], and Dagang Bay [56], and has been recognized as a dominant member of the macrobenthic community near the Northeast Fujian NPP [13,36,67] (Table 5). Its blockage risk is driven by three key biological traits. First, it lacks developed locomotive organs and possesses a soft, highly flexible body wall [68], allowing it to pass through the 5 mm screens typically used in NPP cooling systems—unlike larger, rigid-bodied Echinoderms (e.g., sea urchins). Second, its 100% floating capacity enables passive transport by currents toward the water intake, increasing the probability of screen contact. Third, its high proportional biomass (11.75–53.66% during medium-risk periods) means that even moderate population increases can lead to substantial screen accumulation.
Notably, the maximum GMRI value for Protankyra bidentata recorded here (64.98%) is considerably higher than the 46.34% (low risk) reported by Cai et al. [12] and Lin et al. [56]. This discrepancy may be linked to elevated nutrient levels in 2019, which promoted organic matter accumulation in surface sediments [69], thereby creating favorable habitat conditions that supported a population expansion of Protankyra bidentata. This finding connects nutrient-driven community changes directly to the risk of biological blockage.
In contrast, Actiniaria sp. presented only an episodic medium risk, with a GMRI of 54.63% recorded in July 2021. Its blockage mechanism is distinct: rather than physical accumulation, it relies on viscous secretions from its tentacles to adhere to screen surfaces [70]. These secretions form stable biofilms that directly impede water flow and can trap other small organisms (e.g., juvenile crustaceans), exacerbating blockage. The episodic nature of this risk suggests that it is triggered by short-term environmental factors, such as seasonal reproductive peaks of Actiniaria sp. or temporary nutrient enrichment that enhances mucus production. This pattern aligns with previous observations that the abundance of sea anemones often increases during summer and autumn [71], likely reflecting seasonal variations in key environmental drivers like temperature and nutrient availability.
4.3. Effects of Habitat Factors on Macrobenthic Communities
The macrobenthic community structure is fundamentally governed by a suite of abiotic habitat factors, a principle demonstrated across diverse coastal systems where factors such as salinity, nutrient loading, and sediment properties are key determinants [72]. Studies in regions like Laizhou Bay and Xiangshan Bay have shown community sensitivity to shifts in salinity and direct responses to nitrogen and phosphorus enrichment [73,74]. In estuarine systems like the Scheldt, nutrients can indirectly shape communities by altering sediment conditions [75], while near coastal infrastructure, factors including suspended solids are often primary drivers [40]. Our long-term study aligns with this established framework and identifies the specific environmental drivers operative in the NPP-adjacent ecosystem.
The Mantel test and random forest analysis identified dissolved inorganic nitrogen and phosphorus as the dominant environmental correlates of the macrobenthic community structure from 2018 to 2024. The significant positive correlation between polychaete abundance and nutrient levels provides the mechanistic basis for their persistent dominance. Elevated nutrients stimulate phytoplankton production, increasing the flux of labile organic matter to the seabed. This enrichment preferentially benefits opportunistic, deposit-feeding polychaetes such as Notomastus cf. aberans and Heteromastus filiformis, fueling their proliferation and numerical dominance [76,77].
Notably, nutrients (NH4+, NO3−) were a key predictor of community diversity, explaining 13.6% of the variance in the Shannon–Wiener index. This points to a process of competitive exclusion under eutrophic conditions: enhanced availability of NH4+ boosts primary production, supporting high densities of a few nutrient-tolerant polychaete species that can outcompete more sensitive taxa, thereby reducing overall community evenness and species richness [76].
This elucidated nutrient–community linkage establishes a conceptual bridge between environmental conditions and operational risk. The same nutrient dynamics that structure the overall community also indirectly modulate habitat suitability for specific, morphologically specialized blockage-risk species. For instance, periods of high nutrient loading can promote sedimentary organic matter accumulation [76], potentially creating favorable conditions for species like Protankyra bidentata, explaining its elevated GMRI in high-nutrient years. Therefore, monitoring key nutrients (NH4+, NO3−) serves a dual purpose: a proxy for general community state and a potential early-warning indicator for conditions that may elevate the biofouling risk posed by specific taxa.
Our study has limitations, including the potential for annual sampling to miss seasonal variations and the absence of a control site. Future work should strengthen high-frequency monitoring, develop integrated predictive models, and implement proactive management strategies based on mechanistic insights into key environmental drivers.
5. Conclusions
This study advances the understanding of NPP ecological impacts by demonstrating the co-dominance of thermal and nutrient drivers in shaping macrobenthic communities over a multi-year scale. The identification of Protankyra bidentata and Actiniaria sp. as medium-risk species highlights the importance of non-dominant, morphologically suited taxa in cooling system blockages. Our results provide a scientific basis for targeted monitoring of these risk species and their environmental drivers (nutrients and temperature). We recommend integrating long-term benthic community data into early-warning NPP risk systems to support proactive management of cooling water system security.
Author Contributions
Conceptualization: W.H.; Methodology: W.H.; Sampling surveys and sample analysis: L.F., D.W., B.Z., S.Y. and Z.Y.; Data analysis and manuscript drafting: W.H. and W.L.; Manuscript revision: W.H. and W.Z. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the Youth Marine Science Fund of East China Sea Bureau, Ministry of Natural Resource, grant number 2025200304, the Key Laboratory of Marine Ecological Monitoring and Restoration Technologies, grant number MEMRT202410, and the Science and Technology Development Fund of the Marine Ecological Joint Research Center of the Coastal Power Plant.
Institutional Review Board Statement
This study did not require ethical approval.
Informed Consent Statement
Not applicable.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.
Acknowledgments
We would like to thank the staff from Ningde Marine Center and Northeast Fujian NPP for their sampling and analysis.
Conflicts of Interest
The authors Zefeng Yu and Shouwei Yu were employed by the company Fujian Ningde Nuclear Power Co., Ltd. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as potential conflicts of interest.
References
- Lin, H.; Zhang, S.; Cao, R.; Yu, S.; Bai, W.; Zhang, R.; Yang, J.; Dai, L.; Chen, J.; Zhang, Y.; et al. A Review on the Risk, Prevention and Control of Cooling Water Intake Blockage in Coastal Nuclear Power Plants. Nucl. Eng. Technol. 2024, 56, 389–401. [Google Scholar] [CrossRef] [Scilit]
- Huang, H.; Wu, W.; Li, K. Editorial: Nuclear Power Cooling-Water System Disaster-Causing Organisms: Outbreak and Aggregation Mechanisms, Early-Warning Monitoring, Prevention and Control. Front. Mar. Sci. 2023, 10, 1218776. [Google Scholar] [CrossRef] [Scilit]
- Yao, L.; He, P.; Xia, Z.; Li, J.; Liu, J. Typical Marine Ecological Disasters in China Attributed to Marine Organisms and Their Significant Insights. Biology 2024, 13, 678. [Google Scholar] [CrossRef] [Scilit]
- An, L.; Wang, L.; Ou, D.; Jia, C.; Li, W.; Ding, Y.; You, C.; Liao, J.; Huang, H. The Ecological Mechanisms of Acetes Blooms as a Threat to the Security of Cooling Systems in Coastal Nuclear Power Plants. J. Coast. Conserv. 2021, 25, 55. [Google Scholar] [CrossRef] [Scilit]
- Huang, W.; Zheng, B.; Wen, D.; Wang, F.; Fan, L.; Yu, Z.; Liu, W.; Zhao, S. Community Characteristics and Potential Risk of Nekton in Waters Adjacent to Ningde Nuclear Power Plant in Fujian, China. Biology 2025, 14, 481. [Google Scholar] [CrossRef] [Scilit]
- Wang, X.; Jin, Q.; Yang, L.; Jia, C.; Guan, C.; Wang, H.; Guo, H. Aggregation Process of Two Disaster-Causing Jellyfish Species, Nemopilema nomurai and Aurelia coerulea, at the Intake Area of a Nuclear Power Cooling-Water System in Eastern Liaodong Bay, China. Front. Mar. Sci. 2023, 9, 1098232. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Chen, X.; Lin, Y.; Zhang, S.; Chang, L.; Tang, X.; Xiang, P.; Lin, H. Potential Risk from and Prevention of Phytoplankton Outbreaks in Blocking the Cooling Water System in a Nuclear Power Plant on the Southeast China Coast. Front. Mar. Sci. 2022, 9, 1034876. [Google Scholar] [CrossRef] [Scilit]
- Tang, Z.; Cheng, F.; Jin, X.; Sun, L.; Bao, R.; Liu, Y. An Automatic Marine-Organism Monitoring System for the Intake Water of the Nuclear Power Plant. Ann. Nucl. Energy 2017, 109, 208–211. [Google Scholar] [CrossRef] [Scilit]
- Jones, M. The Unthinkable Fossil of Hope. N. Engl. Rev. 2019, 40, 38–50. [Google Scholar] [CrossRef] [Scilit]
- Chae, J.; Choi, H.W.; Lee, W.J.; Kim, D.; Lee, J.H. Distribution of a Pelagic Tunicate, Salpa Fusiformis in Warm Surface Current of the Eastern Korean Waters and Its Impingement on Cooling Water Intakes of Uljin Nuclear Power Plant. J. Environ. Biol. 2008, 29, 585–590. [Google Scholar]
- Zhang, C.; Guan, C.; Xu, P.; Liu, G.; Xu, Q.; Wang, X.; Zhao, B. Analysis on Risk Organisms for the Cold Source Water of Nuclear Power Plantin the Eastern Waters of Liaodong Bay. Mar. Environ. Sci. 2019, 38, 41–45. [Google Scholar] [CrossRef]
- Cai, L.; Rao, Y.; Zhao, X.; Yang, D.; Lin, J.; Fu, S.; Zhou, X. Two Risk Indices for Benthic Macrofauna Entrapment Evaluation on the Water Intake Systems in Coastal Nuclear Power Plants. J. Appl. Oceanogr. 2022, 41, 655–662. [Google Scholar]
- Tang, Y.F. Study on Typical Disaster-Causing Organisms of Coastal Nuclear Power Operation Safety: Taking Ningde Nuclearpower as an Example; Shanghai Ocean University: Shanghai, China, 2018. [Google Scholar]
- Song, Y.; Wang, T.; Xiong, M.; Yang, S.; Zhang, H.; Ying, J.; Shi, Y.; Zhao, G.; Zhang, X.; Liu, X.; et al. Analysis of the Distribution Characteristics of Jellyfish and Environmental Factors in the Seawater Intake Area of the Haiyang Nuclear Power Plant in China. Biology 2024, 13, 433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Song, Y.P.; Xing, X.F.; Lin, C.K.; Xiong, M.S.; Zhang, X.J.; Zhang, Z.L.; Wu, S.; Zhang, S.M.; Shi, Y.C.; Wu, Z.L.; et al. Advances in the Investigation and Risk Assessment of Cold Source Blockages in Nuclear Power Plants in China. Nucl. Eng. Des. 2024, 420, 112998. [Google Scholar] [CrossRef] [Scilit]
- Fu, Y.; Wang, S.; Meng, W.; Tang, Y.; Wang, S. Flux Measurement of Jellyfish near Hongyanhe Nuclear Power Station Area in Summer by Using Acoustic Methods. J. Dalian Ocean Univ. 2021, 36, 325–333. (In Chinese) [Google Scholar] [CrossRef]
- Wu, F.X.; Gu, Y.G.; Liu, Q.X.; Zhang, S.F.; Rao, Y.Y.; Liu, H.X.; Dai, M.; Wang, Y.G.; Huang, H.-H. Research on the Seasonal Variation of Zooplankton Community in Daya Bay, South China Sea. Front. Mar. Sci. 2023, 10, 1110160. [Google Scholar] [CrossRef] [Scilit]
- Zeng, L.; Chen, G.B.; Wang, T.; Yang, B.; Yu, J.; Liao, X.; Huang, H.H. Acoustic Detection and Analysis of Acetes Chinensis in the Adjacent Waters of the Daya Bay Nuclear Power Plant. J. Fish. Sci. China 2019, 26, 1029–1039. (In Chinese) [Google Scholar]
- Zhang, J.F. Research on Jellyfish Detection in Cold Source Sea Area of Nuclear Power Plant Based on High Resolution Multi-Beam Acoustic Imaging. Digit. Ocean Underw. Warf. 2020, 3, 146–151. (In Chinese) [Google Scholar] [CrossRef]
- Shi, W.Q.; Yuan, S.; Song, L.N.; Zhang, Y.J.; Xu, N.; Liu, X.Q.; Ma, Y.X. A Preliminary Study on Numerical Simulation Warning of the Risk of Ice Blocking in Water Intake of the Hongyanhe Nuclear Power Plant. Mar. Sci. Bull. 2020, 39, 439–446. (In Chinese) [Google Scholar]
- Li, J.; Xu, M.; Lin, J.; Jiang, Y. The Strategies Preventing Particle Transportation into the Inlets of Nuclear Power Plants: Mechanisms of Physical Oceanography. Front. Mar. Sci. 2023, 10, 1100000. [Google Scholar] [CrossRef] [Scilit]
- Gao, W.; Xiong, B.L.; Cai, C.M.; Gong, Y.F.; Lin, Z. Selection and Layout of Marine Organism Prevention Barriers Based on Cold Source Safety Improvement of Nuclear Power Plants. Water Supply Drain. 2017, 53, 1–3. (In Chinese) [Google Scholar] [CrossRef]
- Fu, X.; Du, F.; Pu, X.; Wang, X.; Han, F. Analysis on Critical Factors of Marine Organism Impacts on Water Intake Safety at Nuclear Power Plants. J. Nucl. Eng. Radiat. Sci. 2020, 6, 041101. [Google Scholar] [CrossRef] [Scilit]
- Li, C.; Huo, J.; Song, Y.; Yang, L.; Liu, S. An Integrated Monitoring System for Disaster-Causing Organisms in the Water Intake Areas of Coastal Nuclear Power Plants. Front. Mar. Sci. 2023, 9, 1089699. [Google Scholar] [CrossRef] [Scilit]
- Zheng, Y.; Zhang, R.; Long, Y.; Jiang, X.; Zhu, R.; Xing, J. Review on Development Status of Comprehensive Prevention and Control Technology for Disaster-Causing Floating Bodies at Water Intake of Nuclear Power Plants. Ann. Nucl. Energy 2025, 212, 111087. [Google Scholar] [CrossRef] [Scilit]
- Xu, G.S. Real-Time Detection System for Underwater Disaster-Causing Organisms in Coastal Nuclear Power Plant; Xiamen University: Xiamen, China, 2019. (In Chinese) [Google Scholar]
- Meng, Y.; Hu, L.; Li, J.; Zhang, J. Research on Marine Biological Monitoring Technology to Improve the Cold Source Safety of Nuclear Power Plant. Electr. Saf. Technol. 2019, 21, 33–39. (In Chinese) [Google Scholar]
- Meng, Y.; Guo, X.; Liu, N.; Liu, Y. An Early-Warning and Decision-Support System of Marine Organisms in a Water Cooling System in a Nuclear Power Plant. J. Dalian Ocean Univ. 2018, 33, 108–112. (In Chinese) [Google Scholar]
- Meng, W.; Liu, Y.; Li, J.; Liu, X.; Guo, X.; Cheng, Z. Early warning model for marine organism detection in a nuclear powerplant based on multi-source information fusion technology. J. Dalian Ocean Univ. 2019, 34, 840–845. (In Chinese) [Google Scholar] [CrossRef]
- Huo, J.; Li, C.; Liu, S.; Sun, L.; Yang, L.; Song, Y.; Li, J. Biomass Prediction Method of Nuclear Power Cold Source Disaster Based on Deep Learning. Front. Mar. Sci. 2023, 10, 1100396. [Google Scholar] [CrossRef] [Scilit]
- Fu, X.; Du, F.; Huang, X.; Pei, J.; Zhang, Z.; Xing, X.; Pu, X. Cooling Water Intake System Safety Analysis Based on Impingement Probability. Front. Mar. Sci. 2023, 10, 1133187. [Google Scholar] [CrossRef] [Scilit]
- Guan, C.J.; Wang, K.; Tian, X.H.; Xu, P.; Lu, H.L.; Liu, Y.J.; Zhao, H.H.; Kong, F. Numerical Simulation of Algae Drifting Path in the Sea Area near Nuclear Power Plant Based on Buoy Observation Data. J. Appl. Oceanogr. 2022, 41, 229–239. (In Chinese) [Google Scholar]
- He, L.Y.; Sun, X.X.; Yu, F.; Wang, K.; Song, S.Q.; Yu, Z.M. Potential Risk and Prevention of Phytoplankton Outbreak to Water-Cooling System in Nuclear Power Plant in Fangchenggang, Guangxi. Oceanol. Limnol. Sin. 2019, 50, 700–706. (In Chinese) [Google Scholar] [CrossRef]
- Hu, S.; Zhang, C.; Liu, Q.; Li, T.; Huang, H.; Liu, S. Short-Term Responses of Phytoplankton Size-Fractionated Structure and Photosynthetic Physiology to Thermal Effluent in a Subtropical Coastal Bay. Front. Mar. Sci. 2023, 10, 1102686. [Google Scholar] [CrossRef] [Scilit]
- Lou, Q.; Zhang, X.; Xiang, X.; Yu, F.; Xiong, Y.; Li, Z. Analysis on the Dynamic Mechanism of Acetes Aggregation near a Nuclear Power Cooling Water System Based on the Lagrangian Flow Network. Front. Mar. Sci. 2023, 10, 1100802. [Google Scholar] [CrossRef] [Scilit]
- Cheng, H. Research on the Causes, Prevention and Control Measures of Bio-Blogging on Nuclear Power Cold Source by Acaudina molpadioidea; Shanghai Ocean University: Shanghai, China, 2018. (In Chinese) [Google Scholar]
- He, Y.L.; Liu, S.H.; Yuan, Y.M.; Jiang, K.J.; Wang, T.; Qin, Y.T.; Ren, Y.H. The potential suitability habitat prediction of Acaudina molpadioides based on Maxent model. Acta Oceanol. Sin. 2021, 43, 65–74. (In Chinese) [Google Scholar]
- Deng, B.P.; Liu, H.; Wang, H.B.; Qin, Y.T.; Xia, L.H.; Li, Y.; Zhang, H.F.; Jiang, X.S.; Yang, Y.Y.; Wang, Y.T.; et al. Analysis on the community characteristics and potential ecological risk of jellyfish in the Qingchuan Bay of Ningde, Fujian Province. Acta Oceanol. Sin. 2020, 42, 128–136. (In Chinese) [Google Scholar] [CrossRef]
- Shen, Z.; Fang, W.; Yu, Z.; Chen, X.; Su, Z.; Yu, W.; Lin, H. Key Environmental Parameters and Numerical Prediction Model of Jellyfish Bloom in Qingchuan Bay Nuclear Power Plant, China. Mar. Environ. Res. 2024, 202, 106786. [Google Scholar] [CrossRef] [Scilit]
- Zhang, W.B.; Sun, W.; Xu, X.; Wang, H.B.; Zheng, B.Q.; Lu, C.; Li, J.; Mu, J.L. Ecological environment and the potential hazard-causing organisms in the sea area near the nuclear power plant. Mar. Sci. 2022, 46, 32–43. (In Chinese) [Google Scholar] [CrossRef]
- Zhang, Z.; Shi, Z.; Yu, Z.; Zhou, K.; Lin, J.; Wu, J.; Mu, J. Spatio-Temporal Variations of Zooplankton and Correlations with Environmental Parameters around Tiaowei Island, Fujian, China. Int. J. Environ. Res. Public Health 2022, 19, 12731. [Google Scholar] [CrossRef] [Scilit]
- Liu, W.; Yu, Z.F.; Zhang, Z.; Lin, J.; Cheng, H.; Fan, L.J.; Wang, F.P.; Mu, J.L. Fish assemblage structure and spatio-temporal variation in Qingchuan bay, Ningde, Fujian. Mar. Environ. Sci. 2022, 41, 738–744. (In Chinese) [Google Scholar] [CrossRef]
- Zhao, X.; Cai, L.; Rao, Y.; Yang, D.; Zhou, X.; Wang, D.; Mei, K. Comparison of Macrozoobenthic Communities and Environmental Variables in the Subtidal Zones between a Nearly Closed Bay and an Open Bay. Reg. Stud. Mar. Sci. 2024, 73, 103464. [Google Scholar] [CrossRef] [Scilit]
- Appeltans, W.; Decock, W.; Vanhoorne, B.; Hernandez, F.; Bouchet, P.; Boxshall, G.; Fauchald, K.; Gordon, D.P.; Poore, G.C.B.; Van Soest, R. The World Register of Marine Species: An Authoritative, Open-Access Web-Resource for All Marine Species. 2011. Available online: https://documentatiecentrum.watlab.be/imis.php?module=ref&refid=206211 (accessed on 12 May 2025).
- Liu, R.Y. Checklist of Marine Biota of China Seas; Science Press: Beijing, China, 2008. [Google Scholar]
- GB 17378.4-2007; Marine Monitoring Specifications—Part 4: Seawater Analysis. China Standards Press: Beijing, China, 2007.
- Shannon, C.E.; Weaver, W. The Mathematical Theory of Communication; University of Illinois Press: Urbana, IL, USA, 1963. [Google Scholar]
- Margalef, R. Information Theory in Ecology. Gen. Syst. 1958, 3, 36–71. [Google Scholar]
- Pielou, E.C. Species-Diversity and Pattern-Diversity in the Study of Ecological Succession. J. Theor. Biol. 1966, 10, 370–383. [Google Scholar] [CrossRef] [Scilit]
- Xu, Z.L.; Chen, Y.Q. Relationship Between Aggregation Intensity of Dominant Zooplankton Species and Mackerel-Scad Fishing Grounds in the East China Sea and Yellow Sea in Autumn. Chin. J. Ecol. 1989, 8, 13–15. (In Chinese) [Google Scholar]
- Collins, M.; Tills, O.; Turner, L.M.; Clark, M.S.; Spicer, J.; Truebano, M. Moderate Reductions in Dissolved Oxygen May Compromise Performance in an Ecologically-Important Estuarine Invertebrate. Sci. Total Environ. 2019, 693, 133444. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Galic, N.; Hawkins, T.; Forbes, V.E. Adverse Impacts of Hypoxia on Aquatic Invertebrates: A Meta-Analysis. Sci. Total Environ. 2019, 652, 736–743. [Google Scholar] [CrossRef] [Scilit]
- Leng, Q.; Mohamat-Yusuff, F.; Mohamed, K.N.; Zainordin, N.S.; Hassan, M.Z. Impacts of Thermal and Cold Discharge from Power Plants on Marine Benthos and Its Mitigation Measures: A Systematic Review. Front. Mar. Sci. 2024, 11, 1465289. [Google Scholar] [CrossRef] [Scilit]
- Burrows, M.T.; Bates, A.E.; Costello, M.J.; Edwards, M.; Edgar, G.J.; Fox, C.J.; Halpern, B.S.; Hiddink, J.G.; Pinsky, M.L.; Batt, R.D.; et al. Ocean Community Warming Responses Explained by Thermal Affinities and Temperature Gradients. Nat. Clim. Change 2019, 9, 959–963. [Google Scholar] [CrossRef] [Scilit]
- Friedland, K.D.; Morse, R.E.; Manning, J.P.; Melrose, D.C.; Miles, T.; Goode, A.G.; Brady, D.C.; Kohut, J.T.; Powell, E.N. Trends and Change Points in Surface and Bottom Thermal Environments of the US Northeast Continental Shelf Ecosystem. Fish. Oceanogr. 2020, 29, 396–414. [Google Scholar] [CrossRef] [Scilit]
- Lin, X.C.; Cai, L.Z.; Yang, D.Y.; Zhao, X.Y.; Lin, J.X.; Zhou, X.P. Potential Risk Assessment of Macrozoobenthos Blocking Nuclear Power Cold Source System in Three Subtidal Zone of Fujian, Guangdong and Hainan Coasts. Mar. Environ. Sci. 2023, 42, 286–293. (In Chinese) [Google Scholar]
- Zhou, W.; Yang, Y.; Han, W.; Song, C.; Meng, Z.; Zhang, H.; Han, Q. Effects of Thermal Discharge on the Structuring of Macrobenthic Biological Traits around the Sanmen Nuclear Power Plant in the East China Sea. Mar. Pollut. Bull. 2025, 213, 117705. [Google Scholar] [CrossRef] [Scilit]
- Zhou, W.; Yang, Y.; Han, W.; Huang, A.; Han, Q. Temperature-Gradient Drives Shifts in Macrobenthic Communities near Nuclear Power Plant Thermal Discharges: A Case Study from the Sanmen Bay. Mar. Environ. Res. 2026, 213, 107670. [Google Scholar] [CrossRef] [Scilit]
- Yu, O.H. Spatial Variation in Macrobenthic Communities Affected by the Thermal Discharge Volumes of a Nuclear Power Plant on the East Coast of Korea. Ocean Polar Res. 2013, 35, 299–312. [Google Scholar] [CrossRef] [Scilit]
- Hines, J.; Pereira, H.M. Biodiversity: Monitoring Trends and Implications for Ecosystem Functioning. Curr. Biol. CB 2021, 31, R1390–R1392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Magurran, A.E.; Baillie, S.R.; Buckland, S.T.; Dick, J.M.; Elston, D.A.; Scott, E.M.; Smith, R.I.; Somerfield, P.J.; Watt, A.D. Long-Term Datasets in Biodiversity Research and Monitoring: Assessing Change in Ecological Communities through Time. Trends Ecol. Evol. 2010, 25, 574–582. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Menger, J.; Magagna, B.; Henle, K.; Harpke, A.; Frenzel, M.; Rick, J.; Wiltshire, K.; Grimm-Seyfarth, A. FAIR-EuMon: A FAIR-Enabling Resource for Biodiversity Monitoring Schemes. Biodivers. Data J. 2024, 12, e125132. [Google Scholar] [CrossRef] [Scilit]
- Cai, L.; Rao, Y.; Zhao, X.; Yang, D.; Zhou, X.; Wang, D.; Yue, X. Spatial and Seasonal Distributions of Ten Species of Benthic Macrofauna and Twelve Water Environmental Factors in a Subtidal Zone near the Daya Bay Nuclear Power Plant. Front. Mar. Sci. 2023, 9, 1093468. [Google Scholar] [CrossRef] [Scilit]
- Wang, J.; Liu, Q.; Zhang, C.; Wang, Y.; Yang, F.; Zhao, Y.; Jiang, Y. Microplastics Shift Macrobenthic Community Structures near a Coastal Nuclear Power Plant under Construction in North East China. J. Hazard. Mater. 2022, 437, 129335. [Google Scholar] [CrossRef] [Scilit]
- Wu, H.Y.; Fu, S.F.; Cai, X.Q.; Chen, Q.H. Community Composition and Distribution Characteristics of Macrobenthic Invertebrates in the Subtidal Zone of Major Bays in Fujian Province. Chin. J. Appl. Ecol. 2019, 30, 4240–4248. (In Chinese) [Google Scholar] [CrossRef]
- Du, F.Y.; Wang, X.H.; Jia, X.P.; Yang, S.Y.; Ma, S.W.; Chen, H.G.; Li, C.H. Species Composition and Characteristic Species of Macrobenthos in Daya Bay. J. Fish. Sci. China 2011, 18, 877–892. (In Chinese) [Google Scholar]
- Cheng, H.; Wang, J.H.; Tang, Y.F.; Zheng, B.Q.; Lu, C. Community Characteristics of Macrobenthic Animals and Environmental Quality Analysis in the Coastal Waters of Northern Fujian in Spring. J. Shanghai Ocean Univ. 2018, 27, 238–249. (In Chinese) [Google Scholar]
- Liao, Y.L. Fauna Sinica: Phylum Echinodermata, Class Holothuroidea; Science Press: Beijing, China, 1997. (In Chinese) [Google Scholar]
- Lenzi, M.; Renzi, M. Effects of Artificial Disturbance on Quantity and Biochemical Composition of Organic Matter in Sediments of a Coastal Lagoon. Knowl. Manag. Aquat. Syst. 2011, 402, 08. [Google Scholar] [CrossRef] [Scilit]
- de Orte, M.R.; Clowez, S.; Caldeira, K. Response of Bleached and Symbiotic Sea Anemones to Plastic Microfiber Exposure. Environ. Pollut. 2019, 249, 512–517. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lombardi, M.R.; Lesser, M.P. The Annual Gametogenic Cycle of the Sea Anemone Metridium Senile from the Gulf of Maine. J. Exp. Mar. Biol. Ecol. 2010, 390, 58–64. [Google Scholar] [CrossRef] [Scilit]
- Dijkstra, J.A.; Mello, K.; Sowers, D.; Malik, M.; Watling, L.; Mayer, L.A. Fine-scale Mapping of Deep-sea Habitat-forming Species Densities Reveals Taxonomic Specific Environmental Drivers. Glob. Ecol. Biogeogr. 2021, 30, 1286–1298. [Google Scholar] [CrossRef] [Scilit]
- Zhou, H.; Er, H.; Zhang, Z.N. Community Structure of Macrobenthos in Laizhou Bay and Adjacent Waters. Period. Ocean Univ. China 2010, 40, 80–87. (In Chinese) [Google Scholar] [CrossRef]
- Liao, Y.; Shou, L.; Jiang, Z.; Tang, Y.; Du, P.; Zeng, J.; Chen, Q.; Yan, X.; Chen, J. Effects of Fish Cage Culture and Suspended Oyster Culture on Macrobenthic Communities in Xiangshan Bay, a Semi-Enclosed Subtropical Bay in Eastern China. Mar. Pollut. Bull. 2019, 142, 475–483. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fang, X.; Mestdagh, S.; Ysebaert, T.; Moens, T.; Soetaert, K.; Colen, C.V. Spatio-Temporal Variation in Sediment Ecosystem Processes and Roles of Key Biota in the Scheldt Estuary. Estuar. Coast. Shelf Sci. 2019, 222, 21–31. [Google Scholar] [CrossRef] [Scilit]
- Lin, J.; Zou, X.; Huang, F. Effects of the Thermal Discharge from an Offshore Power Plant on Plankton and Macrobenthic Communities in Subtropical China. Mar. Pollut. Bull. 2018, 131, 106–114. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Benelli, S.; Bartoli, M. Worms and Submersed Macrophytes Reduce Methane Release and Increase Nutrient Removal in Organic Sediments. Limnol. Oceanogr. Lett. 2021, 6, 329–338. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.