


Simple Summary
Since its introduction to China in 1991, Argopecten irradians concentricus has become a pillar species in Beibu Gulf aquaculture. This study examined the effects of stocking density and culture site on growth in breeding populations, compared their growth performance and genetic diversity within control populations, and identified optimal culture locations. Environmental analysis revealed Beihai (BH) exhibited narrower fluctuations in salinity, pH, and dissolved oxygen; total algal abundances were 155,370 cells∙L−1 (BH), 931 cells∙L−1 (QZ), and 47,957 cells∙L−1 (FCG), with Chaetoceros dominant in BH and FCG, and Pleurosigma dominant in QZ. Growth experiments demonstrated a significant negative correlation between growth rate and stocking density, while QZ populations exhibited significantly higher mortality. Breeding populations showed superior growth performance, but lower genetic diversity compared to controls. FCG was identified as a suitable site for cultivating breeding populations, with these findings providing a reference for understanding the species’ aquaculture management strategies and genetic diversity in the region.
Abstract
Argopecten irradians concentricus has become one of the pillar industries in the aquaculture of the Beibu Gulf since it was introduced into China in 1991. This study examined how stocking density and culture site affects growth in breeding populations, compared their growth performance and genetic diversity within control populations, and identified optimal culture locations for A. i. concentricus in the Beibu Gulf. The environmental investigation results revealed that among the three aquaculture sites of Beihai (BH), Qinzhou (QZ) and Fangchenggang (FCG), the fluctuation ranges of salinity, pH, and dissolved oxygen at the BH site were relatively narrower. The sum of all algal genus abundances of the three sites were 155,370 cells∙L−1, 931 cells∙L−1, and 47,957 cells∙L−1, respectively. Chaetoceros was the sole dominant algal genus in both BH and FCG, while Pleurosigma was the only dominant genus in QZ. The experimental results of growth demonstrated a significant negative correlation between growth rate and stocking density (p < 0.05). The mortalities of the QZ populations were significantly higher than those of the BH and FCG populations (p < 0.05). In comparison with the control populations, the breeding populations exhibited better growth performance but lower genetic diversity. FCG is a suitable location for cultivating the breeding population of A. i. concentricus. The findings of this study can serve as a reference for further understanding of the aquaculture strategy and genetic diversity of A. i. concentricus in the Beibu Gulf, China.
1. Introduction
Argopecten irradians concentricus, which is naturally distributed along the Atlantic coasts of the United States and the Gulf of Mexico, is a eurythermal species with a temperature range of 13–33 °C [1]. It was introduced to China in 1991 and since been widely cultured in southern China [1]. The Beibu Gulf, located in the northwest of the South China Sea, is a major aquaculture area for mollusk aquaculture [2,3]. In 2002, A. i. concentricus began to be promoted and bred in the Beibu Gulf and achieved remarkable success [4]. However, the profitability of the scallop industry decreased sharply due to its high mortality, slow growth, and frequent occurrence of diseases, presumably resulting from severe inbreeding in the last decade [5]. To address this and with the purpose of genetic improvement, Liu et al. [6] initiated selective breeding on it in 2007. After continuous generations of selection and breeding, a genetically stable breeding population was obtained.
Currently, studies on A. i. concentricus genetic breeding [7,8], artificial breeding [5,9], the effects of environmental factors on individuals [10,11], and the development and characterization of microsatellite loci [12,13] have been reported. These studies have provided foundations for the cultivation of A. i. concentricus in the Beibu Gulf of China. For the aquaculture of A. i. concentricus in China, the feeding environment and stocking mode are important factors influencing productive performance. Bivalves, which feed on phytoplankton, zooplankton, and suspended solids, are significantly influenced by these food sources in terms of their survival and growth [14]. Previous studies on the stocking density of Meretrix lyrata [15], Haliotis discus hannai Ino [16], Mizuhopecten yessoensis [17], Chlamys farreri [18], and Pinctada martensi [19] have revealed that stocking density has significant impacts on the growth rate and mortality of shellfish, and a reasonable density can greatly enhance breeding efficiency. Nevertheless, there has been no report on the optimum stocking density of A. i. concentricus in the Beibu Gulf of China. Exploring appropriate breeding environments and stocking densities can further promote the development of A. i. concentricus aquaculture.
This study aims to assess the effects of stocking density and sites on the growth traits of the breeding population of A. i. concentricus. Additionally, we compared the growth traits and genetic diversity between the breeding population and the control populations to assess the growth performance of the breeding population. The results of this study may offer a theoretical basis for the directional and rational expansion of the production scale of the A. i. concentricus industry in the Beibu Gulf.
2. Materials and Methods
2.1. Experimental Sites and Scallops
The experimental sites set along the coast of the Beibu Gulf in China, were Beihai (BH, 21°01′ N, 109°06′ E), Qinzhou (QZ, 21°40′ N, 108°42′ E), and Fangchenggang (FCG, 21°31′ N, 108°14′ E), respectively. The scallop breeding population employed in this experiment comprised the eighth selected generation (G8) derived through successive selective breeding. In contrast, the three control populations were founded via artificial breeding using non-selected scallop broodstock cultured at the three respective locations. The breeding group and the control group were jointly bred in a nursery in Zhanjiang, Guangdong. After a specific time interval, they were gathered and transferred to the experimental sites concurrently.
2.2. Growth Experiment
The effect of different culture conditions on growth in different scallops’ strains at the nursery stage and the adult stage, were compared. The stocking density gradient referenced the research and production practices of other cultured scallop species in China [20,21]. The nursery culture stage took place from December 2015 to February 2016. At each of the given sites, both the breeding group and the control group were cultivated in cylindrical lanterns furnished with six layers of substrates [14]. The stocking densities were set at 100, 200, and 300 scallops per layer, with six replicates established for each density. The hanging culture depth was around 1.5 m beneath the water surface, and the hanging culture lanterns were spaced approximately 1 m apart. Upon the conclusion of the nursery culture stage, scallops possessing a shell length and shell height of approximately 30 mm were chosen for the adult stage aquaculture experiment. The stocking densities for this stage were 30, 45, and 60 scallops per layer, while the other conditions remained consistent with those of the nursery culture stage. The adult culture stage was carried out from March 2016 to June 2016. On a monthly basis during the experimental period, all scallops were counted, weighed, and their shell height, shell length, and shell width were measured. Subsequently, they were continuously reared until the end of the experiment. Additionally, one extra lantern with the same density as the experimental group was utilized to replace the dead scallops [14,22].
2.3. Environmental Factor and Phytoplankton Analysis
During the aquaculture period, monthly investigations were carried out on the environmental factors and phytoplankton at the three sites. The specific measurement methods for pH, dissolved oxygen, and other parameters, as well as the identification and counting methods of phytoplankton, were in accordance with those described by Wei et al. [14].
2.4. DNA Isolation and PCR Amplification
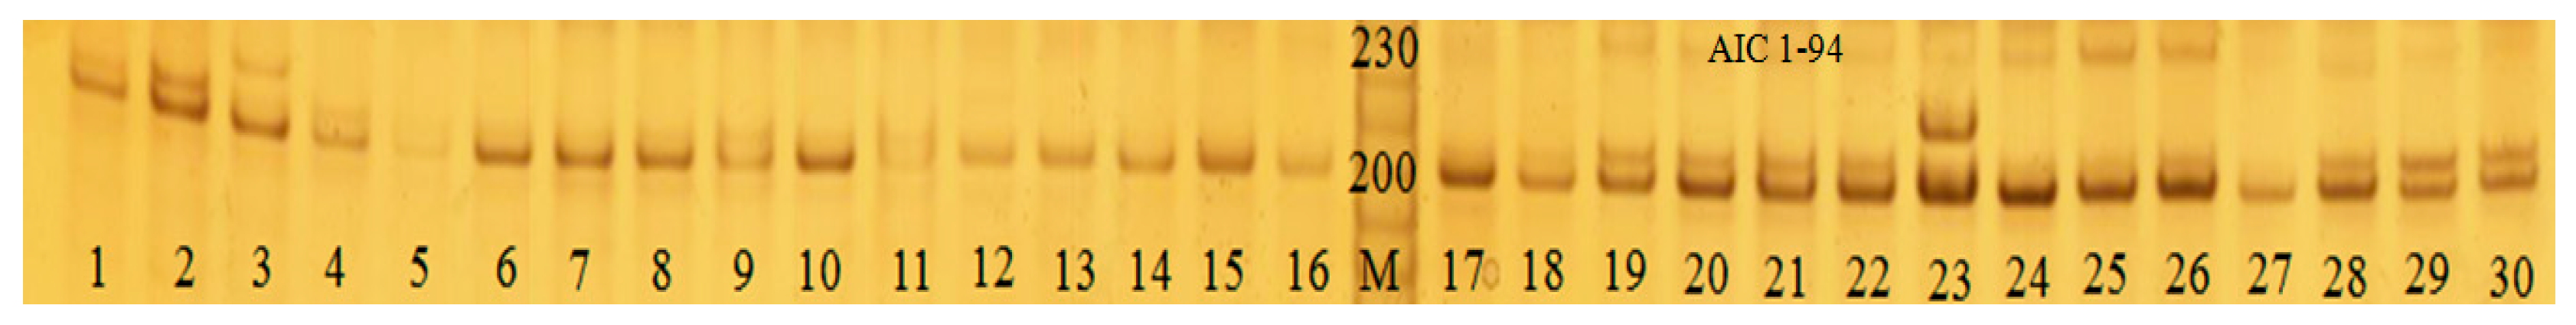
Upon the completion of the growth experiment, 30 scallop muscle samples were randomly collected from each of the six populations, respectively, and then preserved in absolute ethanol. Genomic DNA was extracted using the traditional proteinase K and phenol-chloroform extraction method [23]. The primers were cited from Hu et al. [13], and the basic information is presented in Table 1. The total volume of PCRs was 10 μL, which consisted of 5 μL Taq Mix (Trans Gen, Beijing, China), 2 μL ddH2O, 1 μL of each primer (10 μM), and 1 μL DNA. The reaction procedure was as follows: initial denaturation at 94 °C for 3 min, followed by 35 cycles of denaturation at 94 °C for 45 s, annealing at a primer-specific temperature for 45 s, extension at 72 °C for 45 s, and a final extension at 72 °C for 5 min. Non-denaturing polyacrylamide gel (8%) was employed for the electrophoresis detection of the PCR amplification product, with comparison to the 10 bp DNA ladder (Figure 1). After silver nitrate staining, the results were screened using a gel scanner (Bio-Rad, Hercules, CA, USA).
Table 1.
Information on ten pairs of microsatellite primers.
Figure 1.
Visualization of amplification products from microsatellite locus AIC 1-94 via polyacrylamide gel electrophoresis (representative subset).
2.5. Statistical Analysis
All data were presented in the form of mean ± standard deviation. The statistical analyses were carried out using SPSS Statistics 26.0. Prior to performing the analyses, normality and variance homogeneity of all variables were tested by using Kolmogorov–Smirnov and Levene’s tests, respectively. One-way ANOVA was then conducted, followed by Turkey multiple comparison tests, to compare the growth parameters of the two strains under different stocking densities, as well as to compare the environmental factors at different experimental sites. A p-value of less than 0.05 indicated a significant difference. The correlation analysis of growth traits and stocking density were conducted by Pearson correlation analysis and a two-sided t-test.
Dominant species in the microalgae community are defined as those with a dominance greater than 0.2. The calculation formula of dominance was expressed as: , where Y represents dominance, N represents the total cell abundance of the community, ni represents the cell abundance of i-th species in the community, and fi represents the frequency of the i-th species occurring at each site in the community [14].
Electrophoretic analysis was carried out with Quantity One, and following manual calibration, the size of bands was estimated. The number of alleles (NA), observed heterozygosity (HO), and expected heterozygosity (HE) were computed using Popgen 32.0. The polymorphism information content was determined by Cervus 3.0. MEGA7.0 and was utilized to construct the clustering tree based on the genetic distance between each population.
3. Results
3.1. Effect of Stocking Density, Site, and Strain on the Growth of A. i. concentricus
The harvest data of the nursery and adult culture stages were summarized in Table 2. In general, irrespective of the specific aquaculture site and strain, a significant negative correlation was observed between growth rate and stocking density (p < 0.05). During the nursery culture stage, only when the stocking density was 100 scallops per layer did all the growth traits turn out to be significantly lower than those of the control population (p < 0.05). In the case of the breeding population cultured in FCG, only when the stocking density was 200 scallops per layer were all the growth traits significantly higher than those of the control population (p < 0.05). For the breeding population cultured in QZ, only a certain trait under a specific stocking density was different from that of the control population. For instance, when the stocking density was 200, the breeding population was significantly lower than the control population in terms of body weight (p < 0.05). Regarding the harvest data of the adult stage, under the same site conditions and stocking density, all growth traits of the breeding groups were significantly higher than those of the control groups. (p < 0.05). The breeding population exhibited the fastest growth in FCG and the slowest growth in QZ.
Table 2.
The aquaculture harvest data of the nursery and adult stages of A. i. concentricus.
3.2. Effect of Different Months on the Mortality of A. i. concentricus in Adult Culture Stage
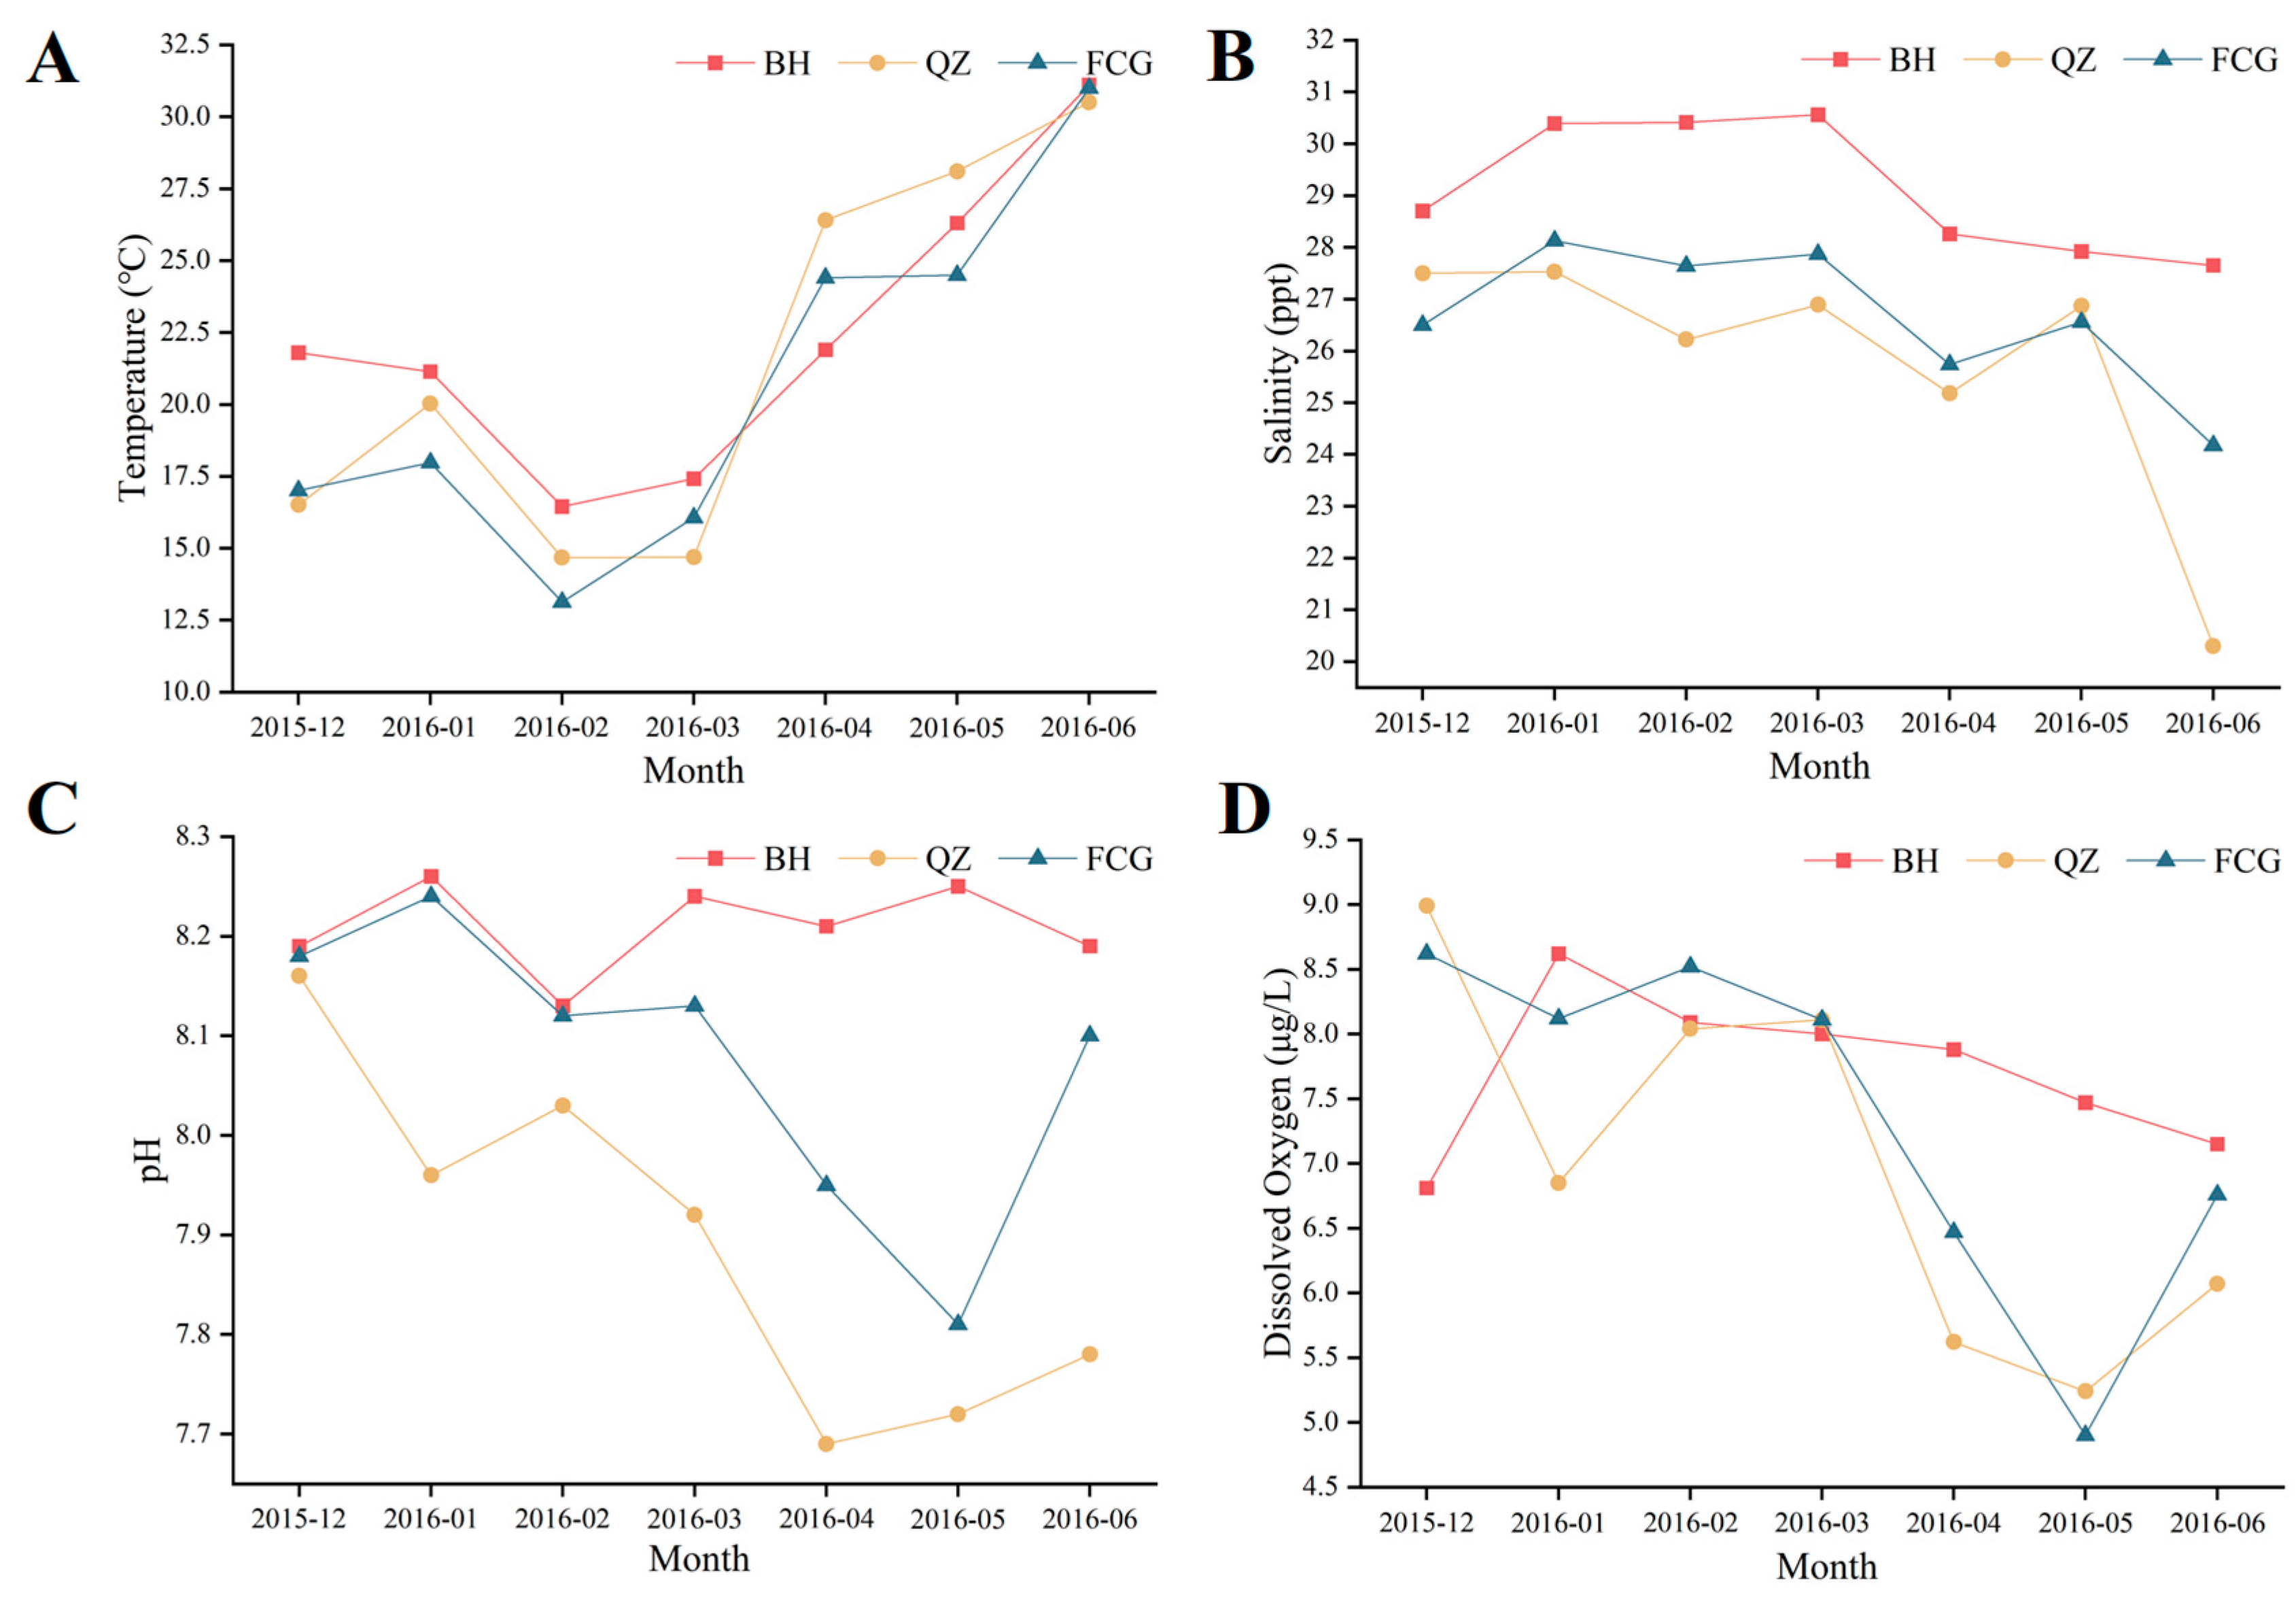
Table 3 presents the mortality situation of scallops in different months during the adult culture stage. For sites, strains, and stocking densities, a sharp increase in mortality was observed in June. This might be attributed to the relatively high seawater temperature in June, as depicted in Figure 2A. Among the different populations, the mortalities of the QZ populations were significantly higher than those of the BH and FCG populations (p < 0.05). For the same site and the same stocking density, no significant differences in mortality were detected between the breeding groups and the control groups.
Table 3.
The mortality data of A. i. concentricus in different months during the adult culture stage.
Figure 2.
The variations in (A) temperature, (B) salinity, (C) pH and, (D) dissolved oxygen at the three cultured sites from December 2015 to June 2016.
3.3. Seawater Quality and Plankton at the Three Sites
Figure 2 illustrates the variations in seawater temperature, salinity, pH, and dissolved oxygen, at the three cultured sites. No significant differences in temperature and dissolved oxygen were found among the three sites, whereas significant differences were present in salinity and pH (p < 0.05). In comparison with QZ and FCG, the fluctuation ranges of salinity, pH, and dissolved oxygen at the BH site were relatively narrower.
A total of twenty-eight, twenty-nine, and twenty-seven genera of phytoplankton were identified at the BH, QZ, and FCG sites, respectively (Table 4). The total abundances of all algal genera at the three aquaculture sites were 155,370 cells∙L−1, 931 cells∙L−1, and 47,957 cells∙L−1, respectively. Chaetoceros was the most abundant algal genus in both BH and FCG and was the only dominant genus. Meanwhile, Pleurosigma was the only dominant genus in QZ. The algae with a 100% occurrence frequency at the aquaculture sites were as follows: Chaetoceros in BH, Coscinodiscus, Pleurosigma, Navicula, Nitzschia in QZ, and Coscinodiscus, Thalassionema, Pleurosigma, Pinnularia, Ceratium furca in FCG.
Table 4.
The phytoplankton genera and their dominance in the three culture sites.
3.4. Genetic Variability of Six Scallop Cultured Populations
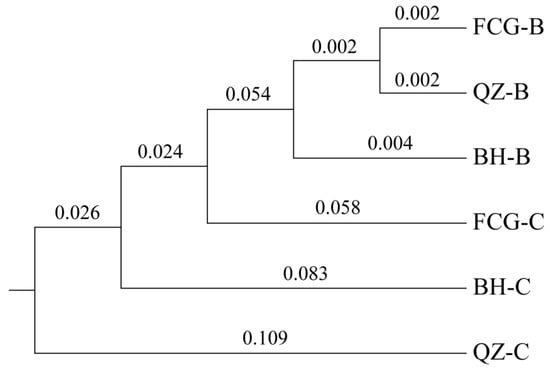
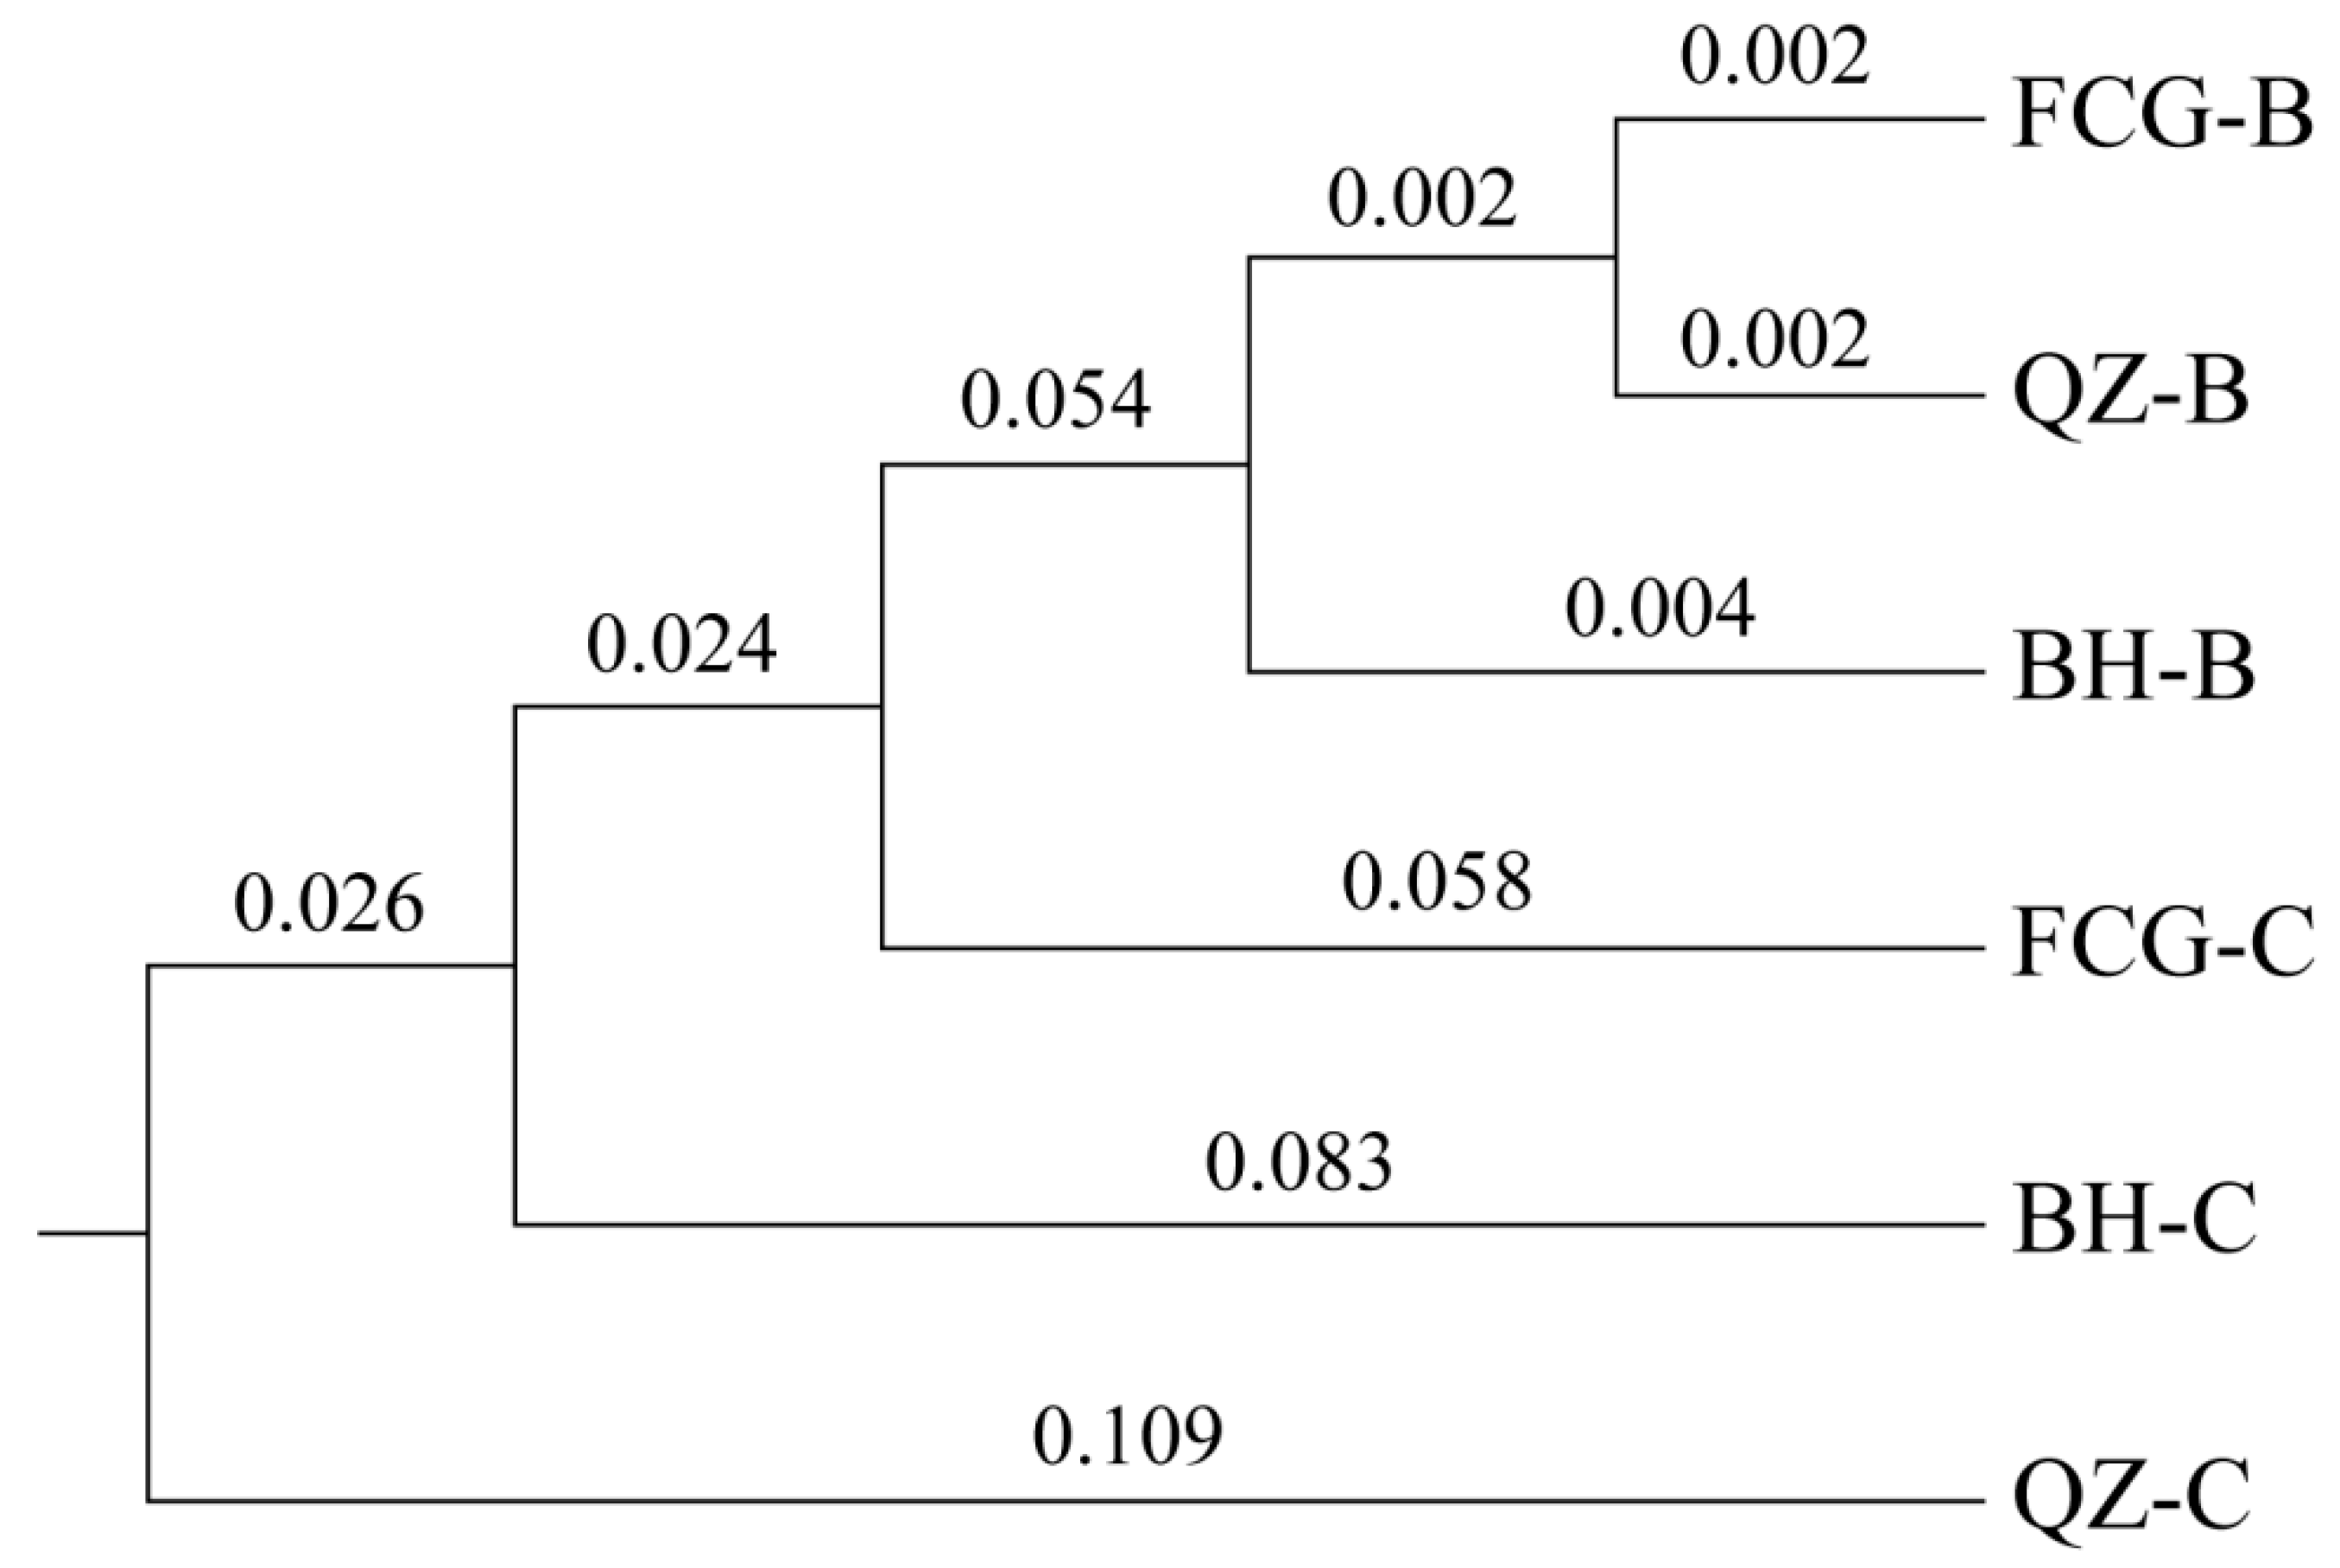
Table 5 presents that the average number of alleles in six scallop populations spanned from 2.80 (BH-B or QZ-B) to 4.40 (BH-C). The average number of effective alleles, average observed heterozygosity, and expected heterozygosity varied from 1.82 (QZ-B) to 3.04 (BH-C), 0.37 (BH-B) to 0.46 (QZ-C), and 0.44 (QZ-B) to 0.62 (BH-C), respectively. With the exception of the control populations at two sites, BH-C and FCG-C, which exhibited high genetic diversity (PIC > 0.5), all other populations displayed moderate genetic diversity (0.25 < PIC < 0.5) [24]. The UPGMA clustering results indicated that the breeding populations BH-B, QZ-B, and FCG-B from the three cultured sites were initially clustered into one group due to their closer genetic distance. Subsequently, the three control populations, FCG-C, BH-C, and QZ-C, were clustered into the group in sequence (Figure 3).
Table 5.
Microsatellite-based genetic variability parameters of six scallop populations.
Figure 3.
The UPGMA clustering tree of six scallop cultured populations based on Nei’s genetic distance. B, Breeding population of A. i. concentricus; C, Control population of A. i. concentricus.
4. Discussion
4.1. Effects of Different Stocking Densities on Growth Performance
The scallop production performance is influenced by numerous factors. These include water temperature [25], salinity [26], attachment organisms [27], aquaculture capacity [28], and culture methods [29], among others. Multiple reports have demonstrated that stocking density significantly impacts the growth of aquatic organisms. High stocking density can lead to food competition, slower growth, and significant size differences [20,21,30]. Due to high stocking density, aquaculture animals have adverse effects on the environment, such as lower dissolved oxygen (DO) and excessive ammonium-nitrogen (NH4–N) [31]. Simultaneously, the deteriorated environment, in turn, affects the growth and survival of aquatic organisms, resulting in a reduced growth rate and increased mortality [31]. Some studies have discovered that mortality may not be affected within a certain density range; however, if the stocking density exceeds a threshold, mortality will rise [32]. Marshall and Dunham [33] conducted a study on the survival rates of Crassostrea gigas and Venerupis philippinarum under different stocking densities and found that at low stocking densities, the mortality rate was low, and there were no significant differences among different stocking densities. In this study, growth experiments on A. i. concentricus were carried out at different densities in various locations. It was found that growth performance decreased remarkably with the increase in stocking density. This is in line with the research findings in Salmo salar [34], Litopenaeus vannamei [30], Pationopecten yessoensis [20], Haliotis discus hannai Ino [16], and Crassostrea nippona [26].
4.2. Effects of Different Sites on Growth Performance
Different environments have a substantial impact on the growth of scallops. The A. i. concentricus is classified as a eurythermal but stenohaline bivalve, with an optimal temperature range of 27.5–30 °C and an optimal salinity range of 28.7–31.3 ppt for its growth [35]. Qinzhou and Fangchenggang are close to the shore and near river estuaries, making them susceptible to the impacts of rainfall and inland runoff. They are particularly prone to abrupt declines in water salinity caused by heavy rainfall. In contrast, the experimental site in Beihai is far from the mainland and thus, less affected. In this study, the mortality rate of the Qinzhou population, regardless of high or low density, was significantly higher than that of the populations in Beihai and Fangchenggang in June, which may be associated with the abrupt decline in salinity at the Qinzhou aquaculture site during this month. The content of organic carbon in water has a significant influence on the growth of filter-feeding shellfish [36], and algae are also a major food source for filter-feeding shellfish [37]. The study found that the phytoplankton abundance in the Qinzhou aquaculture site was significantly lower than that in the Beihai and Fangchenggang aquaculture sites, which may be one of the reasons for the poor growth performance of the population in this region. It is noteworthy that among the three aquaculture sites, the Beihai site exhibits the most stable and optimal water quality for the growth of A. i. concentricus as well as the highest phytoplankton richness; however, its growth performance is slightly inferior to that of the Fangchenggang site, and the underlying reasons for this phenomenon require further investigation.
4.3. Comparison of the Genetic Diversity of Populations
Heterozygosity is a crucial indicator for assessing the genetic diversity of a population [38]. The higher the heterozygosity, the greater the degree of genetic variation. Expected heterozygosity represents the theoretical frequency of heterozygotes when a population is in an equilibrium state. Compared with observed heterozygosity, it can more accurately reflect the genetic diversity level of a population [39]. In this study, in comparison with the three control populations of A. i. concentricus, the expected heterozygosity (HE) and polymorphic information content (PIC) of the selected breeding populations were slightly reduced, suggesting a decrease in the genetic diversity of the selected population during the continuous artificial breeding process.
5. Conclusions
In summary, a significant negative correlation exists between growth rate and stocking density. The breeding populations display better growth performance despite lower genetic diversity in comparison to the control populations. Among the three aquaculture sites, the seawater environment in Beihai exhibits relatively less fluctuation and possesses the highest microalgae diversity. In contrast, the algal genus abundance in Qinzhou is the lowest, and its mortality rate is the highest. The mortality of the Beihai populations and the Fangchenggang populations during the adult culture period are similar. Based on the growth rate, Fangchenggang is determined to be the optimal site for cultivating the breeding populations of A. i. concentricus. The optimal stocking density of scallops is contingent upon the overall cultivation strategy and is consequently influenced by multiple factors such as the desired final market product, market size, and types of growth techniques. Further research remains necessary.
Author Contributions
Q.W.: Writing—original draft. J.F.: Methodology, investigation, data curation, formal analysis, visualization. Y.Q.: Writing—review and editing. Y.P.: Writing—review and editing, supervision, software, resources, funding acquisition, formal analysis. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by the National Natural Science Foundation of China (Grant No. 32260914), the General Project of Guangxi Natural Science Foundation (Grant No. 2025GXNSFAA069872) and the Counterpart Aid Project for Discipline Construction from Guangxi University (Grant No. 2023B03).
Institutional Review Board Statement
The animals in this study were approved by the Animal Care and Use Committee of Guangxi University (Guangxi, China).
Informed Consent Statement
Not applicable.
Data Availability Statement
Data will be made available on request.
Conflicts of Interest
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
References
- Zhang, H.; Liu, X.; Zhang, G.; Wang, C. Growth and survival of reciprocal crosses between two bay scallops, Argopecten irradians concentricus Say and A. irradians irradians Lamarck. Aquaculture 2007, 272 (Suppl. 1), S88–S93. [Google Scholar] [CrossRef] [Scilit]
- Xu, Y.; Zhang, T.; Zhou, J. Historical occurrence of algal blooms in the northern Beibu gulf of China and implications for future trends. Front. Microbiol. 2019, 10, 451. [Google Scholar] [CrossRef] [Scilit]
- Ji, Y.; Yan, G.; Wang, G.; Liu, J.; Tang, Z.; Yan, Y.; Qiu, J.; Zhang, L.; Pan, W.; Fu, Y.; et al. Prevalence and distribution of domoic acid and cyclic imines in bivalve mollusks from beibu gulf, China. J. Hazard. Mater. 2022, 423, 127078. [Google Scholar] [CrossRef] [Scilit]
- Tan, J. Transcriptome Analysis of Argopecten irradians Concentricus and Study on the Molecular Markers Ofits Progeny Crossed with Argopecten bohaihong. Master’s Thesis, Guangdong Ocean University, Zhanjiang, China, 2018. (In Chinese) [Google Scholar]
- Liu, J.; Liu, Z.; Sun, X. The effects of inbreeding on production traits of the southern bay scallop Argopecten Irradians concentricus. J. Shellfish Res. 2011, 30, 109–113. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Wang, H.; Zheng, Y. The effect of parental selection on inbred first filial generation of Argopecten irradians concentricus Say. J. Fish. China 2007, 31, 443–451. (In Chinese) [Google Scholar]
- Yang, C.; Wang, L.; Liu, C.; Zhou, Z.; Xin, Z.; Song, L. The polymorphisms in the promoter of HSP90 gene and their association with heat tolerance of bay scallop. Cell Stress Chaperon. 2015, 20, 297–308. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, X.; Li, C.; Chen, M.; Liu, B.; Yan, X.; Wang, C. Draft genomes of two Atlantic bay scallop subspecies Argopecten irradians irradians and A. i. concentricus. Sci. Data 2020, 7, 99. [Google Scholar] [CrossRef] [Scilit]
- Zheng, H.; Xu, F.; Zhang, G. Crosses between two subspecies of bay scallop Argopecten irradians and heterosis for yield traits at harvest. Aquac. Res. 2011, 42, 602–612. [Google Scholar] [CrossRef] [Scilit]
- Griffith, A.W.; Harke, M.J.; Depasquale, E.; Berry, D.L.; Gobler, C. The harmful algae, Cochlodinium polykrikoides and Aureococcus anophagefferens, elicit stronger transcriptomic and mortality response in larval bivalves (Argopecten irradians) than climate change stressors. Ecol. Evol. 2019, 9, 4931–4948. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yang, B.; Gao, X.; Zhao, J.; Liu, Y.; Xie, L.; Lv, X.; Xing, Q. Summer deoxygenation in a bay scallop (Argopecten irradians) farming area: The decisive role of water temperature, stratification and beyond. Mar. Pollut. Bull. 2021, 173, 113092. [Google Scholar] [CrossRef] [Scilit]
- Li, H.; Liu, X.; Zhang, G. A consensus microsatellite-based linkage map for the hermaphroditic bay scallop (Argopecten irradians) and its application in size-related QTL analysis. PLoS ONE 2012, 7, e46926. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, P.; Liu, H.; Pan, Y.; Qu, Y.; Tian, X.; Wang, K.; Wei, Y.; Wu, X.; Xing, X.; Zhang, Z.; et al. Microsatellite records for volume 11, issue 3. Conserv. Genet. Resour. 2019, 11, 365–368. [Google Scholar] [CrossRef] [Scilit]
- Wei, Z.; Qin, Y.; Liu, H.; Xing, Q.; Yu, Z.; Zhang, Y.; Pan, Y. Aquaculture performance and genetic diversity of a new [(Crassostrea hongkongensis ♀ × C. gigas ♂) ♂ × C. hongkongensis ♀] variety of the oyster “south China No. 1” in Beibu Gulf, China. Biology 2024, 13, 297. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Liu, J.; Mei, S. Effects of tide levelculture density and season on growth and survival of wrinkled clam, Meretrix lyrata, juveniles. Mar. Sci. 2011, 35, 34–41. [Google Scholar] [CrossRef] [Scilit]
- Gao, X.; Zhang, M.; Li, X.; Wu, F.; Song, C.; Liu, Y. Effects of stocking density on survival, growth, and food intake of Haliotis discus hannai Ino in recirculating aquaculture systems. Aquaculture 2018, 482, 221–230. [Google Scholar] [CrossRef] [Scilit]
- Miyoshi, K.; Chiba, S. Predation risk management of sea stars (Asterias amurensis and Distolasterias nipon) by adjusting the density and size of seeded scallops (Mizuhopecten yessoensis): An improvement to local mariculture. Aquacult. Int. 2022, 30, 429–443. [Google Scholar] [CrossRef] [Scilit]
- Xiao, J.; Ford, S.; Yang, H.; Zhang, G.; Zhang, F.; Guo, X. Studies on mass summer mortality of cultured zhikong scallops (Chlamys farreri Jones et Preston) in China. Aquaculture 2005, 250, 602–615. [Google Scholar] [CrossRef] [Scilit]
- He, M.; Zhang, H.; Yuan, T. The growth and survival of a selected line in pearl oyster Pinctada martensii cultured in different densities, water, layers and sites. J. Trop. Oceanogr. 2009, 28, 68–71. [Google Scholar] [CrossRef]
- Liu, S.; Cui, J.; Lin, Y. Effects of self-thinning in the sea of raft culture of Pationopecten yessoensis. J. Fish. China 2013, 37, 1513–1520. (In Chinese) [Google Scholar] [CrossRef] [Scilit]
- Li, Z.; Liu, Z.; Liu, F.; Zhong, Y. Cultured density of new Argopecten irradians concentricus line in nursery and adult culture stage. Oceanol. Limnol. Sin. 2013, 44, 1557–1565. (In Chinese) [Google Scholar]
- De Oliveira, I.B.; Lavander, H.D.; Lima, P.; Oliveira, C.Y.B.; De Dantas, D.M.; Olivera Gálvez, A. Effect of stocking density on the growth and survival of Anomalocardia brasiliana (Gmelin, 1791) (Bivalvia: Veneridae) post-larvae. Cienc. Rural 2019, 49, e20190420. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Ma, W.; Song, X.; Lin, Q.; Gui, J.; Mei, J. Characterization and development of EST-SSR markers derived from transcriptome of yellow catfish. Molecules 2014, 19, 16402–16415. [Google Scholar] [CrossRef] [Scilit]
- Botstein, D.; White, R.L.; Skolnick, M.; Davis, R.W. Construction of a genetic linkage map in man using restriction fragment length polymorphisms. Am. J. Hum. Genet. 1980, 32, 314–331. [Google Scholar]
- Jonasson, J.P.; Thorarinsdottir, G.G.; Eiriksson, H.; Marteinsdottir, G. Temperature tolerance of Iceland scallop, Chlamys islandica (O.F. Muller) under controlled experimental conditions. Aquac. Res. 2004, 35, 1405–1414. [Google Scholar] [CrossRef] [Scilit]
- Wang, T.; Li, Q.; Zhang, J.; Yu, R. Effects of salinity, stocking density, and algal density on growth and survival of Iwagaki oyster Crassostrea nippona larvae. Aquacult. Int. 2018, 26, 947–958. [Google Scholar] [CrossRef] [Scilit]
- Li, Y.; Sunila, I.; Wikfors, G.H. Bioactive effects of Prorocentrum minimum on juvenile bay scallops (Argopecten irradians irradians) are dependent upon algal physiological status. Bot. Mar. 2012, 55, 19–29. [Google Scholar] [CrossRef] [Scilit]
- Liu, X.; Zhang, M.; Wang, Z.; Wang, B. Assessment of bivalve carrying capacities and seeding densities in aquaculture areas of Jiaozhou Bay, China, using ecological modeling and the food balance. J. World Aquacult. Soc. 2021, 52, 1178–1193. [Google Scholar] [CrossRef] [Scilit]
- Grant, J.; Emerson, C.W.; Mallet, A.; Carver, C. Growth advantages of ear hanging compared to cage culture for sea scallops, Placopecten magellanicus. Aquaculture 2003, 217, 301–323. [Google Scholar] [CrossRef] [Scilit]
- Façanha, F.N.; Oliveira-Neto, A.R.; Figueiredo-Silva, C.; Nunes, A.J.P. Effect of shrimp stocking density and graded levels of dietary methionine over the growth performance of Litopenaeus vannamei reared in a green-water system. Aquaculture 2016, 463, 16–21. [Google Scholar] [CrossRef] [Scilit]
- DiMaggio, M.A.; Ohs, C.L.; Broach, J.S.; Sink, T.D. Effects of Stocking Density on Growth, Survival, and Stress Physiology of Pigfish. N. Am. J. Aquacult. 2014, 76, 201–210. [Google Scholar] [CrossRef] [Scilit]
- Iguchi, K.I.; Ogawa, K.; Nagae, M.; Ito, F. The influence of rearing density on stress response and disease susceptibility of ayu (Plecoglossus altivelis). Aquaculture 2003, 220, 515–523. [Google Scholar] [CrossRef] [Scilit]
- Marshall, R.D.; Dunham, A. Effects of culture media and stocking density on biofouling, shell shape, growth, and survival of the Pacific oyster (Crassostrea gigas) and the Manila clam (Venerupis philippinarum) in suspended culture. Aquaculture 2013, 406–407, 68–78. [Google Scholar] [CrossRef] [Scilit]
- Calabrese, S.; Nilsen, T.O.; Kolarevic, J.; Ebbesson, L.O.E.; Pedrosa, C.; Fivelstad, S.; Hosfeld, C.; Stefansson, S.; Terjesen, B.; Takle, H.; et al. Stocking density limits for post-smolt Atlantic salmon (Salmo salar L.) with emphasis on production performance and welfare. Aquaculture 2017, 468, 363–370. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.G.; Liu, J.Y.; Wang, H.; Zheng, Y.L. Study on adaptability of juveniles of Argopecten irradians concentricus say to salinity. J. Zhanjiang Ocean Univ. 2006, 26, 12–16. (In Chinese) [Google Scholar]
- Li, H.M.; Zhang, Y.Y.; Liang, Y.T.; Chen, J.; Zhu, Y.C.; Zhao, Y.T.; Jiao, N. Impacts of maricultural activities on characteristics of dissolved organic carbon and nutrients in a typical raft-culture area of the Yellow Sea, North China. Mar. Pollut. Bull. 2018, 137, 456–464. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lage, S.; Costa, P.R.; Moita, T.; Eriksson, J.; Rasmussen, U.; Rydberg, S.J. BMAA in shellfish from two Portuguese transitional water bodies suggests the marine dinoflagellate Gymnodinium catenatum as a potential BMAA source. Aquat. Toxicol. 2014, 152, 131–138. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Q.; Yu, H.; Yu, R. Genetic variability assessed by microsatellites in cultured populations of the Pacific oyster (Crassostrea gigas) in China. Aquaculture 2006, 259, 95–102. [Google Scholar] [CrossRef] [Scilit]
- Nei, M.; Tajima, F.; Tateno, Y. Accuracy of estimated phylogenetic trees from molecular data. J. Mol. Evol. 1983, 19, 153–170. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).