1. Introduction
In everyday life, individuals must continuously process motion-related information, such as approaching pedestrians or passing vehicles when crossing a street, and make safe behavioral decisions based on this information. In competitive sports, the demands on motion-information processing are even more pronounced (
Scharfen & Memmert, 2019). In table tennis, for example, the ball travels at high speeds, lands unpredictably on multiple points, and exhibits varying degrees of spin. These characteristics place exceptional demands on players’ visual information processing, reaction speed, motor-control precision, and decision-making abilities.
Experience plays a crucial role in enhancing an individual’s capacity to process information. Long-term physical training promotes motor performance, optimizes the visuomotor cortical network, and improves cortical neural efficiency, consistent with the principles of brain plasticity (
Zhang et al., 2025). Prolonged, sport-specific training induces adaptive structural and functional changes in the cerebral cortex, thereby enhancing athletes’ motor skills and cognitive abilities (
Logan et al., 2022). A scoping review with meta-analysis on EEG research found that the favorable brain function in athletes can be summarized as neural efficiency, increased cortical asymmetry, greater cognitive flexibility, and precise timing of cortical activation (
Fang et al., 2022). Therefore, continuous professional skill training can further reshape brain architecture and function (
Zhang et al., 2021), strengthen neural network plasticity, and ultimately improve the processing of motor-related information. Research has shown that elite athletes possess extensive procedural and declarative knowledge, enabling them to extract critical cues from complex environments (
McPherson, 2000). Differences in motor-information processing between athletes and non-athletes are also evident at the neural level. According to the neural efficiency hypothesis (NEH), experts exhibit more efficient cortical functioning during cognitive tasks (
L. Li & Daniel, 2021). For instance, compared with amateurs and young elite, researchers has found that expert table tennis players are characterized by enhanced cortical activation in the motor and fronto-parietal cortex during motor imagery in response to table tennis videos (
Wolf et al., 2014). In addition, elite expert players in table tennis have less activation of the fronto-parietal attention network (
Wolf et al., 2014). Greater neural efficiency is typically reflected in reduced activation of task-relevant brain regions and enhanced inhibition of irrelevant neural activity (
Qiu et al., 2019). In electrophysiological studies, larger P3 amplitudes indicate a greater allocation of cognitive resources to the task at hand (
Key et al., 2005). The N2 component, which appears around 200–400 ms with a frontal-midline maximum, displays more negative amplitude in tasks involving perpetual conflict and response inhibition (
Kousaie & Phillips, 2017). In other word, larger N2 amplitudes are usually associated with enhanced inhibition.
You et al. (
2018) compared response inhibition between table tennis players and non-athletes under both conscious and unconscious conditions. Their findings showed that athletes exhibited larger P3 amplitudes in No-Go trials across both conditions, indicating stronger inhibitory control and higher neural efficiency. Another study reported that during tasks involving motion anticipation and visuospatial memory, high-speed stimuli elicited larger P3 amplitudes; however, the experienced group demonstrated shorter P3 latency, suggesting more rapid working-memory updating and more efficient decision making (
Chueh et al., 2017). A study reported that ERP N2 amplitudes, or N2 or P3 latencies, the elite and expert groups exhibited notably faster reaction times and more pronounced P3 amplitudes than the intermediate group did during the cognitive task (
Chang et al., 2024). Long-term training also strengthens the cerebral cortex’s capacity to regulate motor actions (
Patel & Azzam, 2005). Research has further shown that table tennis players exhibit shorter N2 latency under all conditions, reflecting faster conflict-monitoring processes (
You et al., 2018). Using a masking paradigm, another study examined athletes’ neural efficiency in processing spin-serve information at an unconscious level. The results revealed markedly reduced N2 amplitudes under incongruent conditions, indicating superior conflict monitoring and response-suppression abilities (
Shi et al., 2024).
Huang et al. (
2024) investigated behavioral performance and neural activity in table tennis players during domain-specific (color-word Stroop) and spatially based (spatial Stroop) tasks. They found that athletes displayed lower N2 amplitudes, suggesting that they required fewer neural resources for conflict detection and resolution, evidence that long-term training optimizes the brain’s inhibitory-control network. In general, larger N2 amplitudes reflect heightened cognitive conflict and a greater need for response inhibition.
Taken together, previous research demonstrates that motor experience can enhance neural efficiency and improve the processing of motor-related information. However, studies examining how varying levels of experience influence motor-information processing from the perspective of neural activity remain limited (
Chen et al., 2024). The majority of studies have only compared the behavioral and neural mechanisms between elite athletes and non-athletes within a specific sport (
Moscatelli et al., 2016), or have merely examined the differences between athletes and non-athletes in processing general movement information (
Song et al., 2024). Few studies examined the differences in how elite athletes, amateur athletes, and non-athletes processed sport-related information.
To address this gap, the present study recruited college students with different levels of table tennis experience, including table tennis specialists, athletes from other sports, and non-sports majors, to participate in an electroencephalogram (EEG) experiment. Participants freely viewed a series of images while their electroencephalographic activity was recorded. These images were taken from screenshots of table tennis matches. Competitive images were extracted from the athletes’ official competition period, and non-competitive images were captured from their pre-competition training sessions. Our objective was to investigate the differences in neural responses to competitive and non-competitive images among three distinct groups, in order to elucidate the role of motor experience in the processing of motor-related information. We hypothesize that motor experience would modulate the processing of motion information, reflected in differential N2 and P3 amplitudes across groups. Specifically, table tennis players and ordinary athletes may have extensive training in their specific sports, which results in a smaller amplitude of the P3 component compared to non-athletes. That is to say, they can effectively process sports-related information without requiring a lot of cognitive resources. For the passive viewing of competitive images, since the images are related to the information of table tennis in the competition scene, table tennis players may be more sensitive and show differences in the amplitude of the N2 component compared to non-athletes. The findings of this study are expected to provide empirical support for the NEH.
2. Materials and Methods
2.1. Participants
A two-factor mixed experimental design of 3 (sports experience: table tennis players, ordinary athletes, non-athletes) × 2 (image type: competitive vs. non-competitive) was employed. The required sample size was estimated using G*Power 3.1.9.2 (α = 0.05, 1 − β = 0.90, effect size f = 0.25), indicating a minimum of 54 participants. Ultimately, 60 college students were recruited, with 20 individuals assigned to each group. Table tennis players were required to engage in at least 10 h of professional training per week. This group included 15 male students (M = 21.47, SD = 1.52) and 5 female students (M = 21.60, SD = 1.28). Ordinary athletes, who had no table tennis experience, also trained for no less than 10 h per week. This group comprised 14 males (M = 21.33, SD = 1.50) and 6 females (M = 21.83, SD = 0.41). The non-athlete group consisted of 20 students without any formal sports training experience, including 5 males (M = 21.75, SD = 0.96) and 15 females (M = 21.40, SD = 2.38). All participants were in good physical health, reported no history of psychiatric or neurological disorders, and were right-handed. Before the experiment, written informed consent was obtained from all participants, and they received monetary compensation upon completion of the study. The experimental protocol was approved by the university’s ethics committee (Approval No.: LL2024193).
2.2. Stimuli and Procedure
The experimental materials consisted of 150 images extracted from various table tennis matches. These images were categorized into two conditions: competitive, in which the athlete was depicted in an active competitive state, and non-competitive, in which the athlete was shown in a practice or training context. To validate the categorization, 25 table tennis players who did not participate in the main experiment rated the images. Based on their evaluations, 30 images with low discriminability between competitive and non-competitive states were removed. The final stimulus set comprised 120 images, including 60 competitive and 60 non-competitive pictures. The competitive-state ratings (1–5 scale) showed a significant difference between the two categories, t = 3.68, p < 0.05.
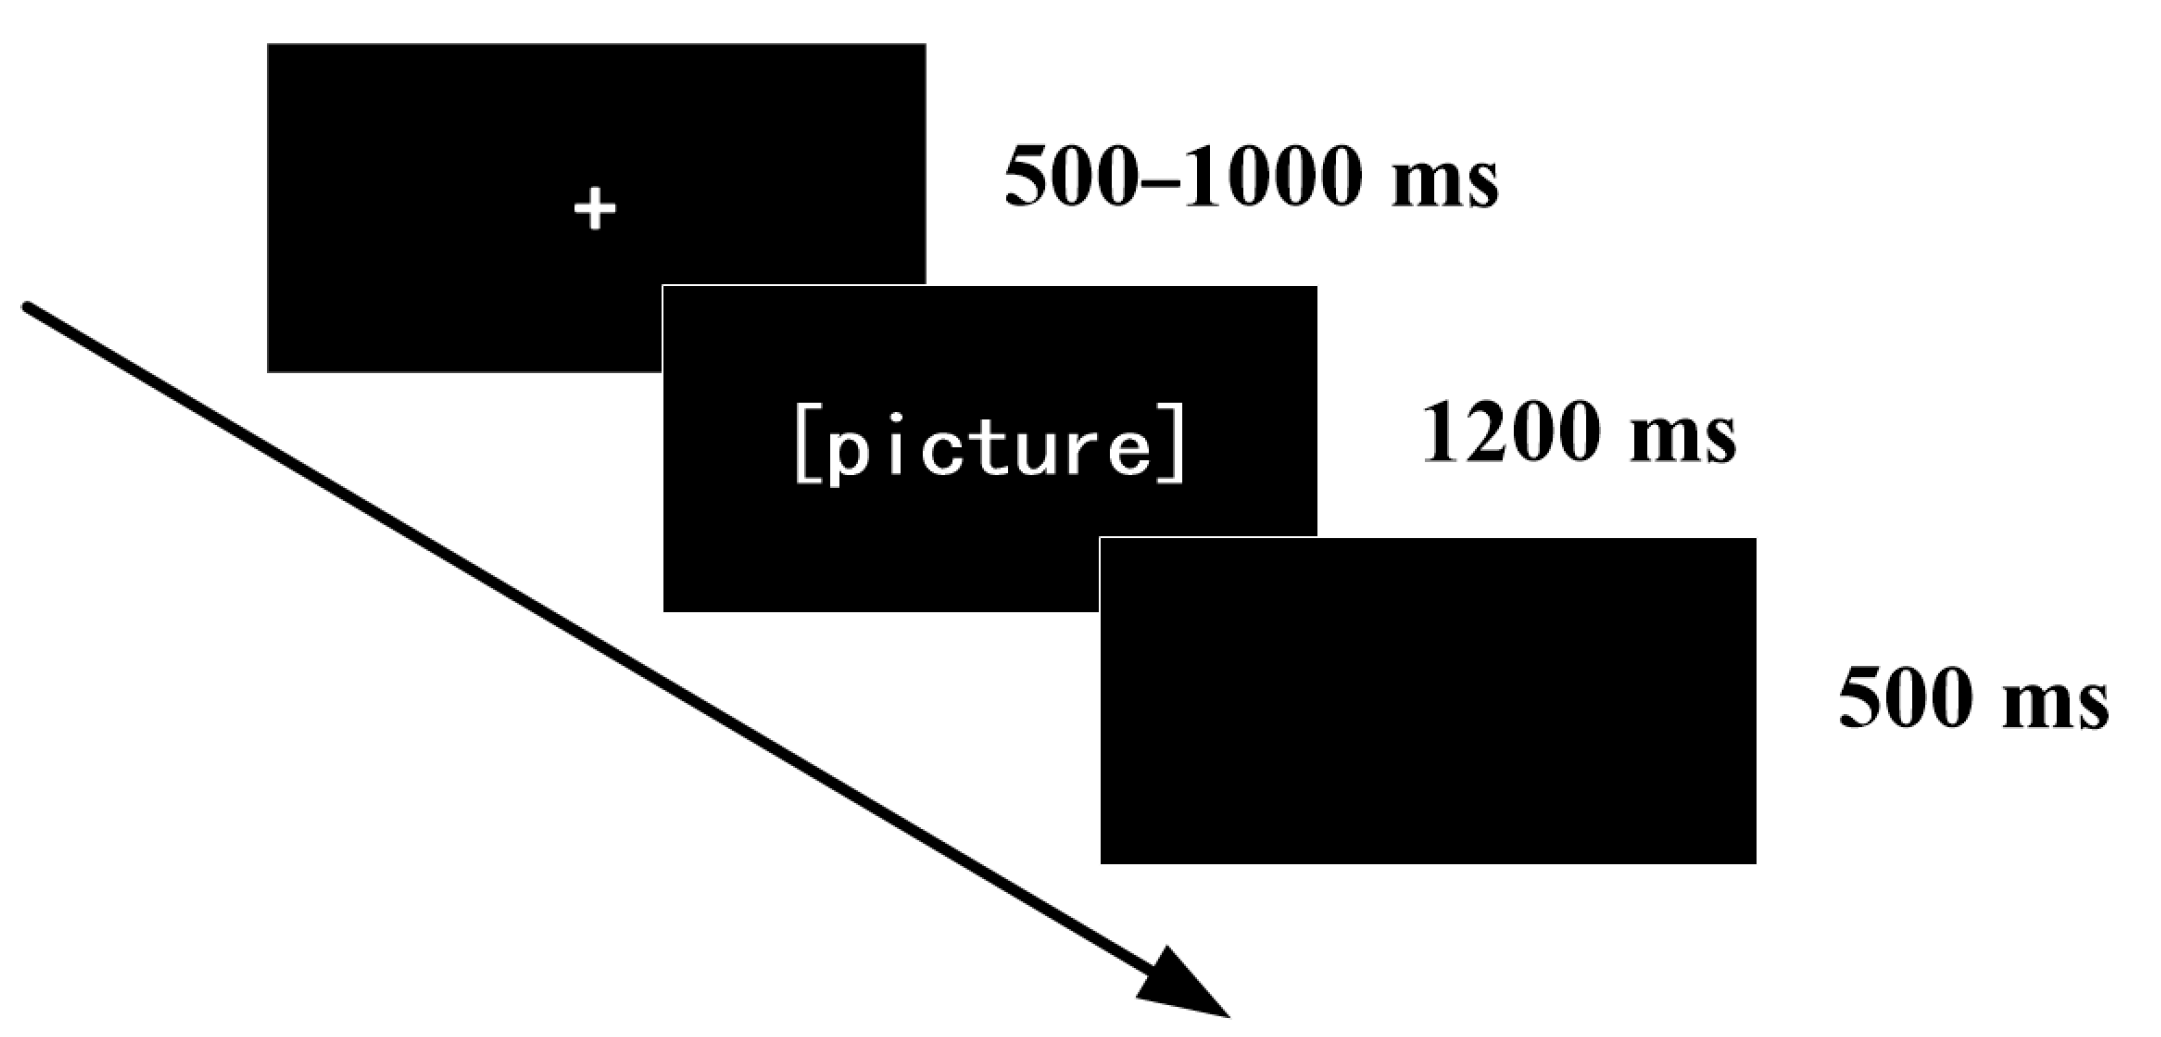
The experiment consisted of two phases. Upon arrival at the laboratory, participants were given a brief rest period, after which the experimenter provided standardized instructions. They then completed eight practice trials to familiarize themselves with the stimulus materials and task procedure. Following the practice phase, the formal experiment began. Each trial started with the presentation of a fixation cross (“+”) for a jittered duration of 500–1000 ms, followed by a table tennis-related image displayed for 1200 ms. Participants were instructed to view each image attentively. After the image disappeared, a blank screen was shown for 500 ms, marking the end of the trial (see
Figure 1). To ensure that the participants would pay close attention to the images, randomly in 20% of the trials, a screen with a question mark appeared after the image was shown, and the participants were required to respond by pressing a “F/J” key to indicate whether the image depicted a competitive state or a non-competitive state. The formal experiment comprised 120 trials in total. The whole experiment was divided into 4 blocks, each block consisting of 30 trials. The participants taken a short break after each block. After adjusting their own state, they would proceed to the next block of the experiment.
2.3. EEG Recording
EEG data were recorded using a 64-channel Brain Products system. Electrode FPz served as the ground, and FCz was used as the online reference. Vertical electrooculogram activity was recorded using an electrode placed below the right eye to monitor blinks and vertical eye movements. Electrode impedances were maintained below 5 kΩ throughout the recording, and EEG signals were digitized at a sampling rate of 1000 Hz.
Offline preprocessing was performed using BrainVision Analyzer 2.0 (Brain Products GmbH, Gilching, Germany). The data were re-referenced to the average of the left and right mastoids and filtered using a 0.1–30 Hz bandpass filter (24 dB/octave). Ocular artifacts were corrected with independent component analysis. The corrected EEG was segmented into epochs from −200 ms to 800 ms relative to stimulus onset, with the −200 to 0 ms interval used for baseline correction. Epochs containing artifacts exceeding ±100 μV in peak-to-peak amplitude were rejected. After artifact removal, the mean numbers of usable trials were as follows: for table tennis players, 50.88 (SD = 6.98) in the competitive condition and 51.41 (SD = 7.11) in the non-competitive condition; for ordinary athletes, 52.68 (SD = 3.87) in the competitive condition and 52.12 (SD = 4.40) in the non-competitive condition; and for non-athletes, 52.06 (SD = 5.72) in the competitive condition and 52.11 (SD = 6.00) in the non-competitive condition.
2.4. Data Analysis
Based on previous studies (
Chueh et al., 2017;
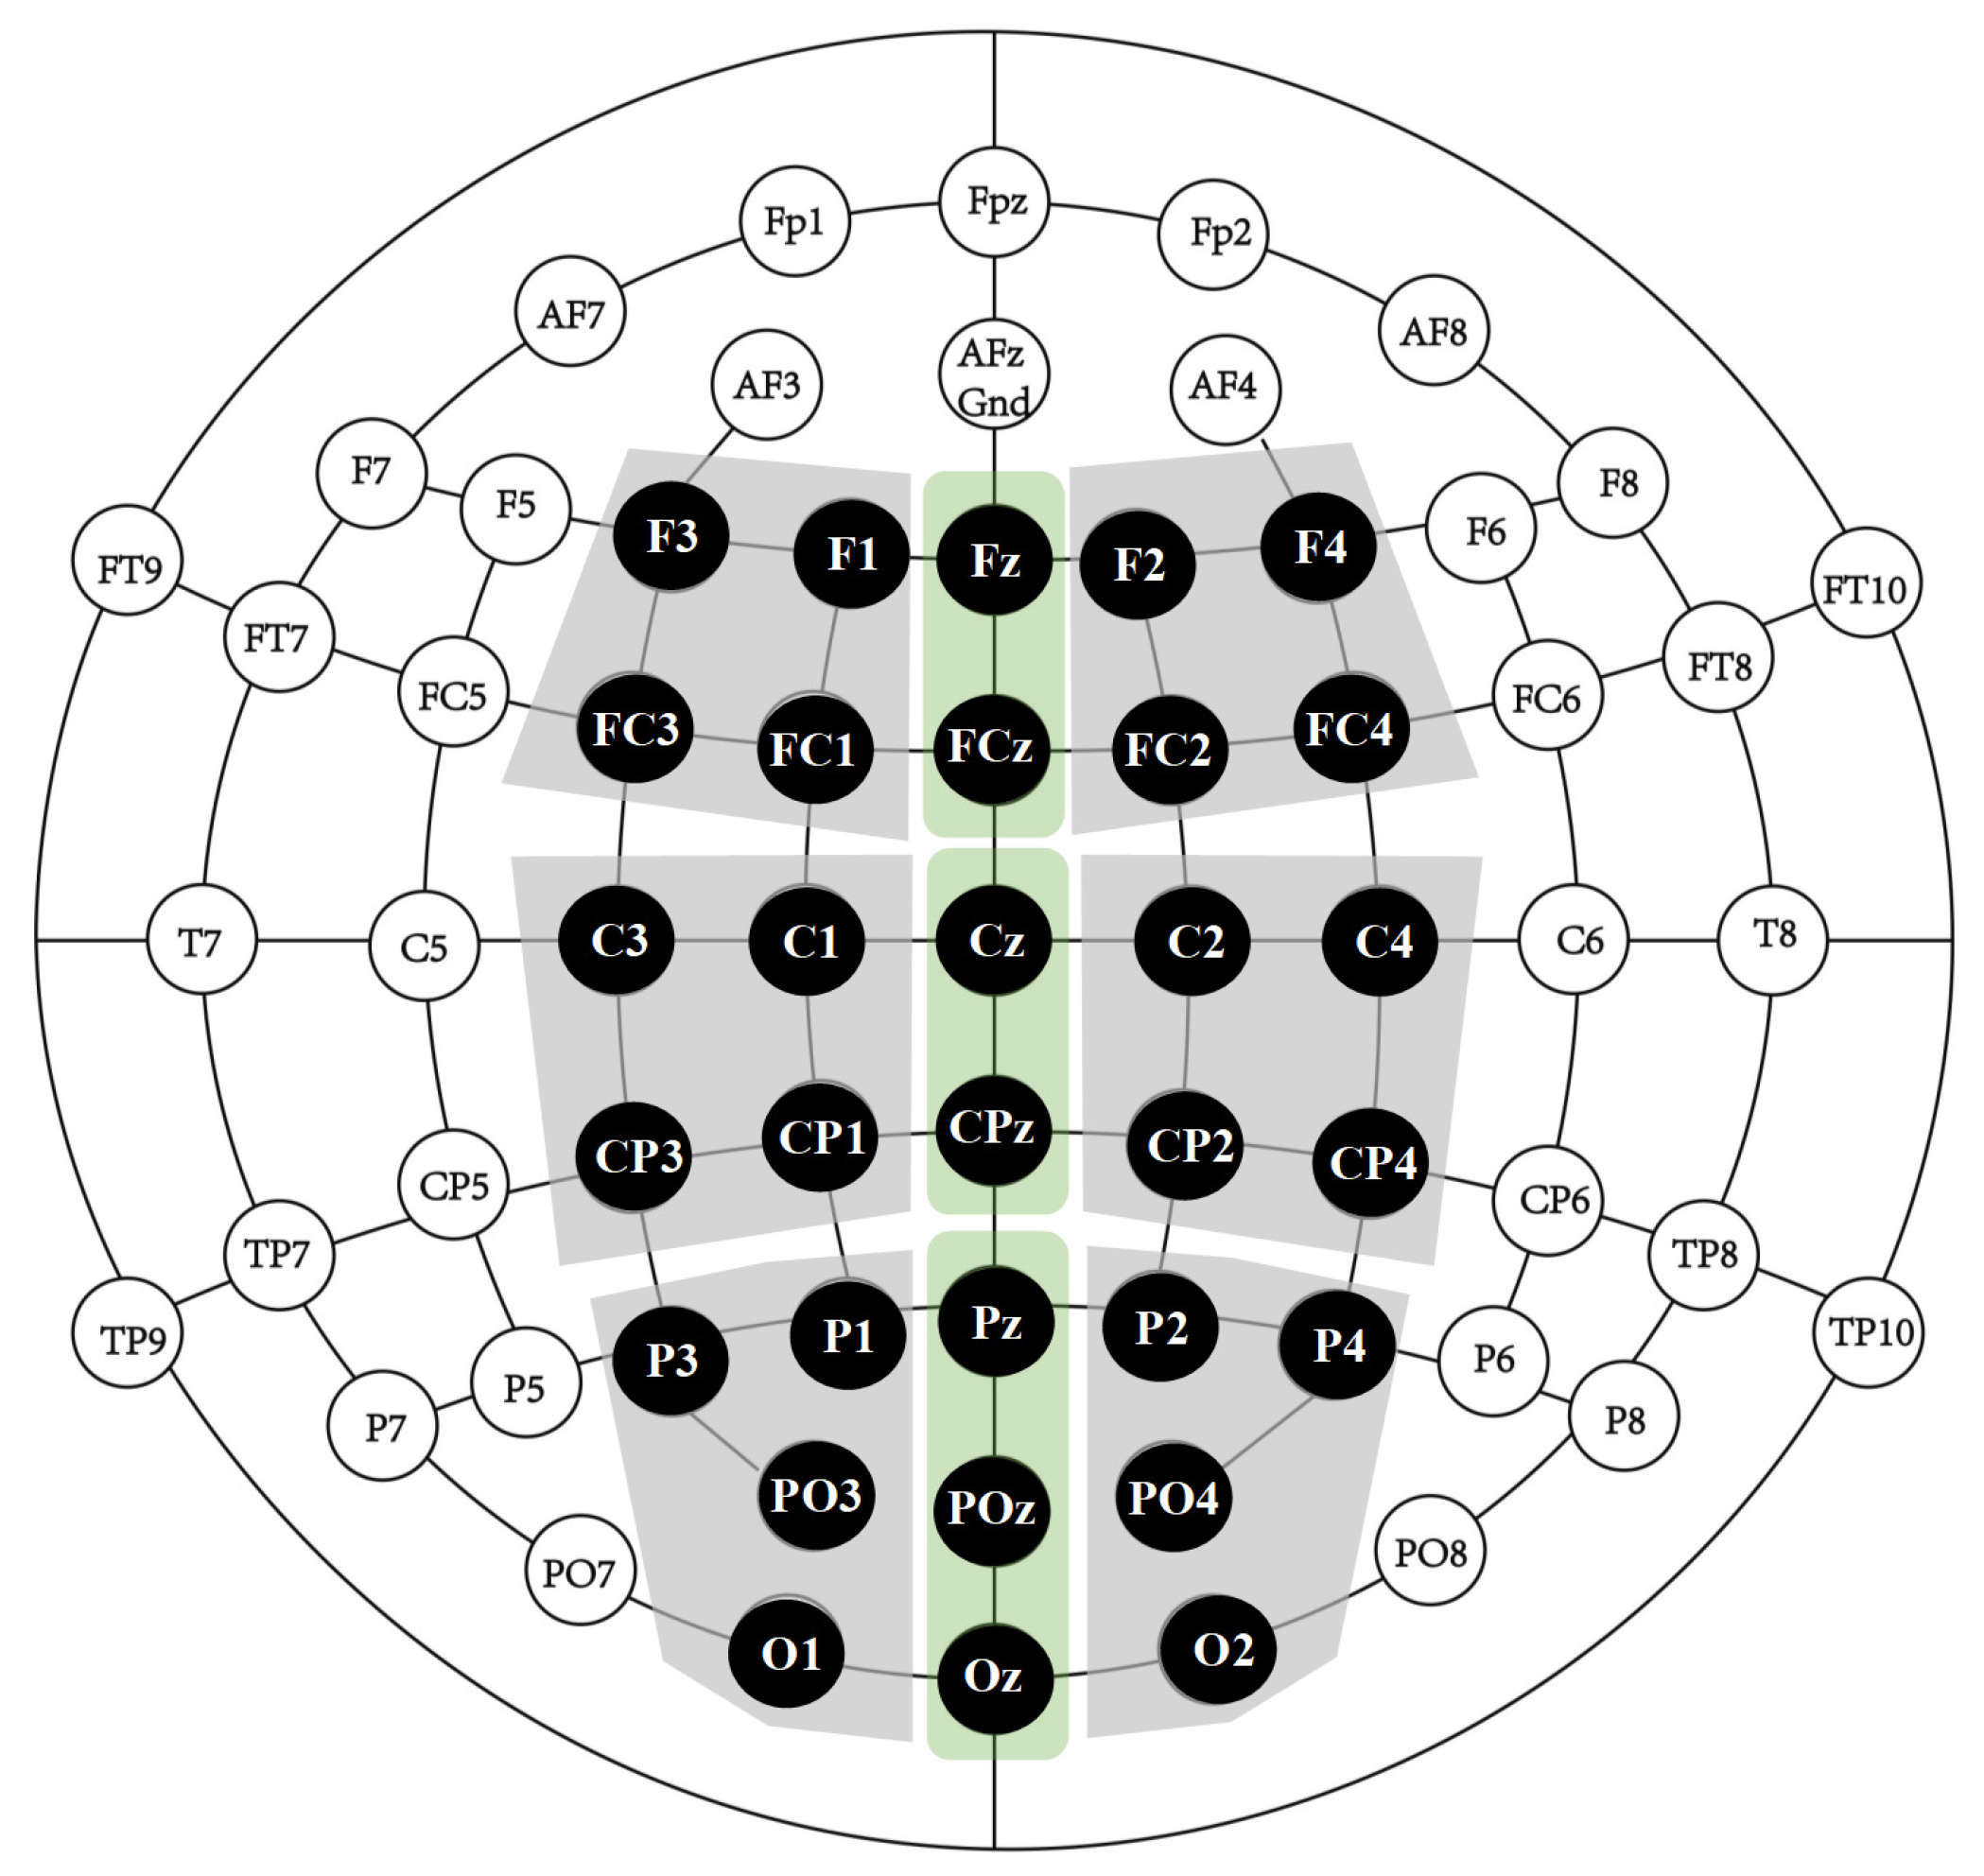
Shi et al., 2024), the N2 component was analyzed within the 220–270 ms time window at frontal and central electrode sites, while the P3 component was analyzed within the 300–460 ms window at central and parietal sites. The regions of interest are illustrated in
Figure 2 and included the following electrode clusters: left-anterior (F1, F3, FC1, FC3), middle-anterior (Fz, FCz), right-anterior (F2, F4, FC2, FC4), left-central (C1, C3, CP1, CP3), middle-central (Cz, CPz), right-central (C2, C4, CP2, CP4), left-posterior (P1, P3, PO3, O1), middle-posterior (Pz, POz, Oz), and right-posterior (P2, P4, PO4, O2).
The N2 amplitudes were analyzed using two separate 3 × 2 × 3 mixed-design ANOVAs with the factors condition (competitive vs. non-competitive) and hemisphere (left, middle, right) as within-subject variables, and group (table tennis players, ordinary athletes, non-athletes) as the between-subject factor. These analyses were conducted separately for frontal and central sites. Similarly, two 3 × 2 × 3 additional mixed-design ANOVAs were conducted on P3 amplitudes for central and posterior sites, respectively, with the same within- and between-subject factors.
For all ANOVAs involving more than one degree of freedom, the Greenhouse-Geisser correction was applied to adjust for violations of sphericity. Post hoc pairwise comparisons were corrected using the Bonferroni method to control for multiple comparisons. Statistical significance was set at an alpha level of 0.05 (two-tailed).
3. Results
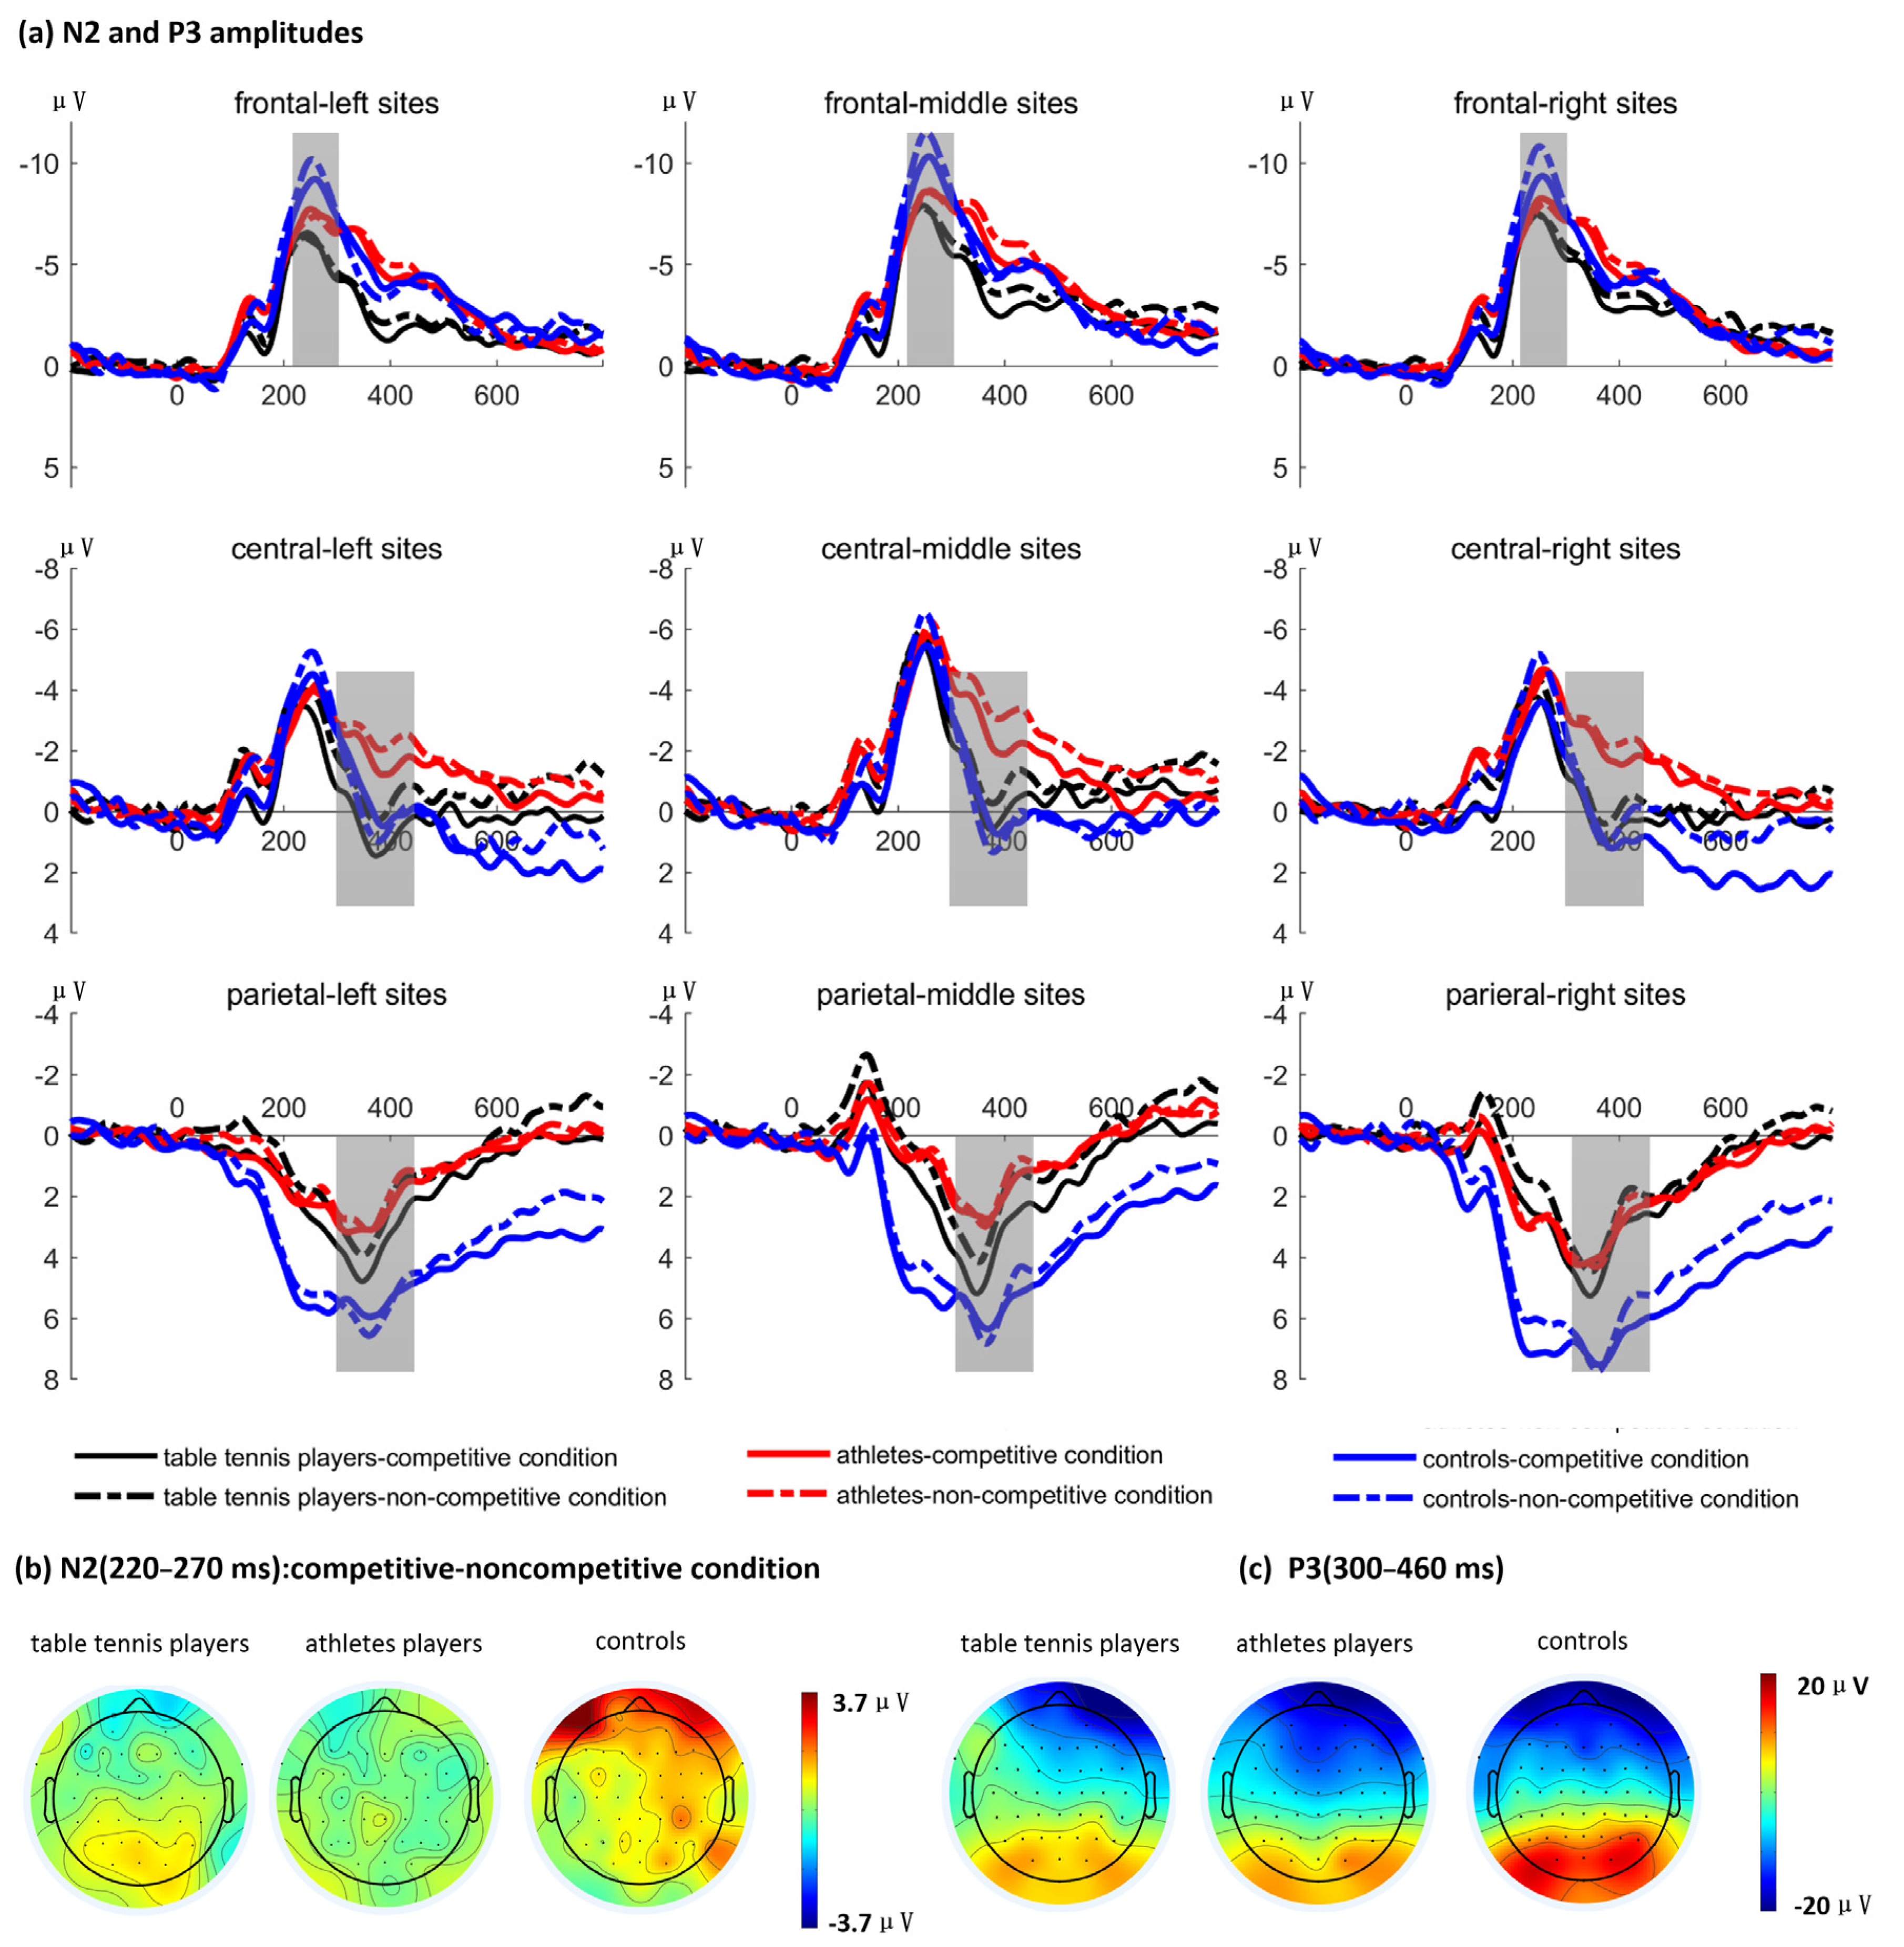
Table 1 showed the average amplitudes of ERPs and
Figure 3 showed the grand average waveforms of ERPs in different sites.
Prior to conducting the repeated-measures ANOVA, the assumption of normality was assessed. we examined the skewness and kurtosis statistics. The absolute values of their corresponding z-scores (calculated by dividing the statistic by its standard error) were all below the critical value of 1.96 for three groups at each condition, indicating no significant departure from normality. The results found that the data within each group at each condition (competitive and non-competitive separately) were normally distributed for N2 amplitudes in frontal sites (all |Z| < 1.82), as well as for P3 amplitude in central (|Z|s < 1.75) and parietal sites (|Z|s < 1.95). Moreover, the data within each group at non-competitive condition were normally distributed for N2 amplitudes in central sites (non-competitive:|Z|s < 1.61). For the competitive condition, although the skewness z-score for the athlete group slightly exceeded the threshold (Z = 2.37), visual inspection of the Q-Q plots indicated an acceptable alignment with the normal distribution. The data of other two groups were normally distributed (|Z|s < 1.89).
3.1. N2 Amplitude
As shown in
Figure 3, a significant interaction between group and condition was observed at the frontal sites,
F (2, 57) = 3.26,
p = 0.046,
ηp2 = 0.10. Post hoc analyses revealed that, for the non-athletes group, the competitive condition elicited significantly smaller N2 amplitudes compared to the non-competitive condition (Δ = 1.17, 95% CI [0.36, 1.97],
p = 0.005). In contrast, no significant differences between conditions were found for either the table tennis players or the ordinary athlete groups (
ps > 0.78). The main effect of group was not significant,
F (2, 57) = 1.42,
p = 0.25, and the main effect of condition did not reach significance,
F (21, 57) = 2.11,
p = 0.15. All other interactions were not significant (
ps > 0.21).
At the central sites, the main effect of condition was significant, F (1, 57) = 6.03, p = 0.02, ηp2 = 0.10, indicating that the competitive condition elicited smaller N2 amplitudes compared to the non-competitive condition. The main effect of group was not significant, F (2, 57) = 0.04, p = 0.97. No other interactions reached significance (ps > 0.07).
3.2. P3 Amplitude
At the central sites, there was a marginally significant main effect of condition, F (1, 57) = 3.93, p = 0.052, ηp2 = 0.06, with the competitive condition eliciting larger P3 amplitudes compared to the non-competitive condition. But the main effect of group was not significant, F (2, 57) = 1.39, p = 0.26. No other significant main effects or interactions were observed (ps > 0.12).
At the parietal sites, a significant main effect of condition was found, F (1, 57) = 4.73, p = 0.034, ηp2 = 0.08, indicating that the competitive condition elicited larger P3 amplitudes than the non-competitive condition. Additionally, there was a significant main effect of group, F (2, 57) = 3.66, p = 0.03, ηp2 = 0.11. Post hoc comparisons revealed that controls elicited larger P3 amplitudes than table tennis players (Δ = 2.77, 95% CI [0.04, 5.50], p = 0.047) and larger amplitudes than ordinary athletes (Δ = 3.50, 95% CI [0.77, 6.23], p = 0.01). No significant difference was observed between table tennis players and athletes (p = 0.60). Other main effects and interactions were not significant (ps > 0.22).