


Simple Summary
In organisms with obligatory sexual reproduction, females are born virgin and need to access male sperm over the course of their life to produce offspring. This problem is simplified in holometabolous insects with complete metamorphosis because food acquisition and sexual activities are segregated into separate life history phases (transition between larval, pupal, and adult stages). Unfortunately, female transition from virgin to mated status in feral populations is challenging to quantify due to the high mobility, small size, and cryptic nature of adult insects. Neotenic female bagworms reproduce within a self-constructed bag, thus providing a model system to parameterize reproductive processes.
Abstract
The probability that female bagworms (Lepidoptera: Psychidae) are in mating time-in (live pheromone calling) was recorded in three bagworm species: Oiketicus kirbyi in a Costa Rican oil palm plantation in 1993–1994; Metisa plana in Malaysian oil palm plantations during five consecutive generations of bagworms in 1996; and Thyridopteryx ephemeraeformis on ornamental trees in the Midwest United States. Because females entirely reproduce within their bag (mate attraction, copulation, and oviposition), it is possible to assess the mating success of time-out females (dead individuals from an ongoing generation that either mated or died as a lifelong virgin) and incidence of calling females that may or may not mate before death. Synchronous larval development and discrete (non-overlapping) generations imply a declining proportion of live calling females over time in all three bagworm species: ‘young’ calling females prevail in the early season as opposed to a majority of time-out (post-reproductive) females in the late season. Calling females are long-lived relative to males (one-day lifespan) and thus expected to mate as adults when abundance of males is high and/or female longevity exceeds three days. A low mating success of calling females is associated with extreme protogyny (early season male shortage; O. kirbyi in 1994) or late adult emergence in populations at the edge of the distribution range (T. ephemeraeformis at latitudes > 41° N in 2019).
1. Introduction
Sexual communication in moths is usually mediated by a female-emitted volatile signal (sex pheromone) for the attraction of males [1,2,3]. Calling females actively releasing pheromone for mate attraction are deemed to be in a mating time-in phase, as opposed to non-calling females who are in a time-out phase [4,5,6,7,8,9]. At the intraspecific level, duration of mating time-in (signalling effort) is amplified for old virgins that call earlier at night and for a longer period than young virgins due to increased risk that females do not mate as adults (matelessness/mating failure/lifelong virginity/zerogamy) [1,10,11,12,13,14].
Polyandry (females mate more than once) implies sequential shifts between mating time-in/time-out during life [15,16]. This problem is simplified in flightless monandrous females that enter a permanent mating time-out phase after successful copulation [17,18,19,20]. With that said, measuring diurnal variation in pheromone emission in large groups of feral females (‘true time-in’: pulsed release of pheromone) is often impractical. In addition, sampling constraints vastly challenge assessment of mating status in feral populations of females owing to the small size/cryptic nature of insects [21,22,23]. The problem is compounded in phenology studies that require repeated observations of mating time-in during the entire emergence season.
The life history of bagworms (Lepidoptera: Psychidae) provides a model system to investigate the incidence of mating time-in due to the unusual tractability of reproduction.
- (1)
- Tractability of populations. Due to conspicuous nature of sessile pupal bags tightly attached onto host plants by larvae before pupation, abundance and demography of bagworms can be assessed in local populations by collecting cohorts of bags at repeated intervals from the onset to the end of the emergence cycle [22,24,25].
- (2)
- Tractability of male and female emergence. Pupae of bagworms exhibit strong sexual dimorphism (♂: obtect pupa; ♀: barrel-shaped pupa; Figure 1 in [26], Figure 6 in [27]) and can be readily sexed by cutting each pupal bag open to examine its content (‘dissection’). Emergence of adult males is indicated by an empty pupal case (or parts thereof) hanging at the lower extremity of the bag; winged males actively seek sexually receptive females. Sessile neotenic females emerge by splitting the anterior segment of their pupal case to expel pheromone-impregnated setae in the lower section of the bag [28,29]. Dissemination of pheromone outside the bag is passive and to some extent independent of female behavior [30,31], thus calling female bagworms are deemed in ‘true’ permanent mating time-in phase when they are alive—with the caveat that attraction does not stop with physiological death of females [30,31].
- (3)
- Tractability of female reproductive status. Female bagworms entirely reproduce within their pupal case inside their bag (attraction of males, copulation, oviposition). The presence of a live female within her split pupal case inside a bag with pheromone-impregnated seta is indicative of an actively calling female; each ‘candidate’ calling female was removed from her pupal case to determine presence/absence of eggs corresponding to either time-out mated females in the process oviposition and ‘true’ virgin calling females, respectively. Among time-out females, the presence/absence of eggs inside pupal cases is a tell-tale sign of mating status [32,33]. Mated females start laying eggs in their pupal case immediately after copulation and die shortly after oviposition is completed [26,34,35,36]. In contrast, the presence of a dead female in a bag with pheromone-impregnated setae but no eggs is indicative of an unmated female that died as lifelong virgin. In sexually reproducing bagworms, unmated females do not lay unfertile eggs in their pupal case, even when close to death [28,35,37].
The life history trajectory of the adult female bagworm is characterized by an obligatory pheromone calling stage (c) followed by one of two scenarios with associated individual reproductive output ř:
ř = Ƒs if c → m
ř = 0 if c → v
Both mated (m) and unmated (v: virgin) females are in time-out (Ŧ: dead females from ongoing generation); average fecundity in any species s is denoted as Ƒs. For any given day i, the reproductive composition of adult populations (Ᾱi) can be summed up as follows:
Ᾱi = n♂i + n♀i (c + mŦ + vŦ)
Considering that time-out females are not available to males for mating, the sex ratio of interest for any day i relates to the number of males per calling female (ᶘi), which is assumed to be positively correlated with hypothetical (post sampling) mating probability of calling females (ci).
ᶘi = ♂i/ci
ci = [mci/(mci + vci)] ᶘi,ȥ
The variables mci and vci represent estimates of calling females that mate or die as lifelong virgins. Rules of thumb to quantify mci/vci relative to ᶘi are detailed in Materials and Methods, including effects of adult longevity (ȥ).
In contrast with time-in females, mating probability among time-out females (Ŧi) can be empirically derived by dissecting pupal bags.
Ŧi = mŦi/Ŧi
Overall female mating success (i) can be approximated by combining Equations (5) and (6).
i = (mŦi + mci)/♀i
Mating functions are bounded between i− and i+, with assumptions that calling females either never or always mate:
i− = mŦi/♀i
i+ = (mŦi + ci)/♀i
The incidence and phenology of calling females (mating time-in) is explored with the Equations above in three species of bagworm [Oiketicus kirbyi Guilding, Metisa plana Walker, Thyridopteryx ephemeraeformis Haworth], factoring latitudinal clines in the latter species. The data set includes >2000 calling females with known sampling dates and locations that are described and analyzed for the first time (Table 1). The data are contextualized noting biological similarities/dissimilarities between species.
Table 1.
Number of adult bagworms (♂, ♀) sampled in Costa Rican and Malaysian plantations of oil palm (Ok: Oiketicus kirbyi and Mp: Metisa plana) and on ornamental host trees in Midwest United States (Te: Thyridopteryx ephemeraeformis). Females were classified as in either mating time-in (c: calling female) or time-out (m, v = mated or virgin females). References as follows for Ok in 1993 [38] and 1994 (published herein for the first time), for Mp in 1996 [39], and for Te in 2007–2009 [22,25,40].
2. Materials and Methods
2.1. Life History of Three Bagworm Species
Oiketicus kirbyi and Metisa plana are defoliators of oil palm, Elaeis guineensis Jacquin, in Central–South America and Southeast Asia (Table 2). Major interspecific differences relate to the short development, small body size, and low fecundity of M. plana relative to O. kirbyi (Table 2): the progeny of one female O. kirbyi has the potential to defoliate leaf areas equivalent to the progeny of 600 female M. plana (Table 3 in [41]). Taxonomically, M. plana and O. kirbyi belong to the subfamilies Metisinae and Oiketicinae (Table 2), with male attraction in both subfamilies involving pheromone impregnated setae shed by females in their bag. The setae shed by emergent female M. plana are reddish in M. plana and bright yellow in O. kirbyi and T. ephemeraeformis. Upon emergence, virgin female Metisinae periodically protrude their head and thoracic segments from the lower section of the bag to further pheromone dissemination and mate attraction; a similar behavior has commonly been observed in old (near death) calling female Oiketicinae [42,43,44].
Table 2.
Summary of life history traits for three bagworm species (Lepidoptera: Psychidae). References for Oiketicus kirbyi: [26,34,38,41,45,46]; for Metisa plana: [36,39,41,47,48]; and for Thyridopteryx ephemeraeformis: [25,33,34,49,50,51,52].
Thyridopterix ephemeraeformis (Oiketicinae subfamily) is native to temperate North America where it defoliates ornamental trees in urban–suburban areas, predominantly Juniperus and Thuja species [53,54]. Body size and fecundity of females is intermediate between M. plana and O. kirbyi (Table 2). Unlike the two other species, T. ephemeraeformis is univoltine with an obligatory overwintering egg stage [55].
2.2. Sampling Procedures
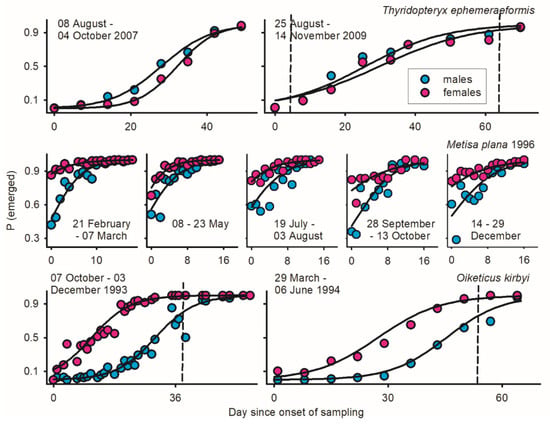
Populations of O. kirbyi were sampled in Costa Rican oil palm plantations during two generations at Coto 50 and Coto 52, approximately 5 km apart (ca 8.62° N 82.98° W). In 1993, pupal bags were collected on all fronds of 170 young palms (3 to 4 m high) at near daily intervals between October 7 and December 3 [38]. The same procedure was used in 1994 by sampling three to nine fronds of 210 ‘old’ palms (4 to 5 m high) at weekly intervals between March 29 and June 6 [39]. Bagworms were sampled from the onset to the end of the emergence cycle (Figure 1). As in any data set below, pupal bags were all cut open to determine the abundance, sex ratio, and reproductive status of females. Early/late season intervals with no calling female (vertical dashed lines in Figure 1) are excluded from analysis.
Figure 1.
Patterns of adult emergence for three species of bagworms [adult/(pupa + adult)] using day since onset of sampling and zero intercept (day i at onset = 0) as time proxy in analysis. (1) Oiketicus kirbyi in plantation of oil palm in Costa Rica in 1993–1994 (Figure 2 in [38]). (2) Metisa plana in Malaysian plantation of oil palm during five consecutive generations in 1996 (G1 to G5) (Figure 5 in [39]). (3) Thyridopteryx ephemeraeformis on ornamental trees in Central Indiana in 2007 [25] and between North Tennessee–South Michigan in 2009 [22]; data in 2008 are not depicted due to short time series of abundance (14 days interval). Parameters of logistic regressions for males and females as provided in Table A1 in Appendix A. Dashed vertical lines represent time intervals with no calling female; these intervals were deleted from subsequent analyses.
Due to the short generation cycle of M. plana combined with sedentary (non-dispersing) larval progeny [41], bagworms from past generations tend to accumulate on old fronds of oil palm. Sampling was thus conducted on one young frond in the upper canopy (<2 months old) which only carried individual bagworms from the ongoing generation. The same palms located in a plantation near Sungei Merah in Peninsular Malaysia were sampled during five consecutive generations of M. plana in 1996. The period of sampling did not cover the entire emergence cycle, focusing instead on the second half of emergence with >50% adult emergence. A sexual segregation of the pupation site (females systematically pupate at higher locations than males: [38,50,51]) is often observed in bagworms, including M. plana [41]. Because only one frond in the upper canopy was sampled, the abundance of males relative to females was multiplied by a conservative factor of two (Table 2 in [41]).
Pupal bags of T. ephemeraeformis were collected in 2007 on infested trees located within a 50 km radius around Lafayette in Indiana (40°–40.5° N) at weekly intervals between August 18 and October 4 [25]. Data in 2008 included 119 sites sampled once between 3 and 16 October within latitudinal range 39.56°–41.28° N [40]. Data in 2009 included 71 sites (up to 9 sampling intervals between 2 September and 14 November) over a wide geographic range (38.39° to 41.74° N) including Tennessee, Kentucky, Indiana, and Michigan (Figure 2 in [22]).
2.3. Data Analysis
All statistical analyses were conducted with the SAS package version 9 (SAS Institute, Cary, NC, USA). Each data set (O. kirbyi in 1993 and 1994; five generations of M. plana in 1996; and T. ephemeraeformis in 2007–2009) was standardized using day i = 0 at the onset of female calling.
The response variable in Equation (4) (ᶘi) is computed as the ratio of males per calling female using average values on a per day basis. Cumulative numbers of males/calling females up to day i (ñ♂i/Ʃ♂i, ñci/Ʃci) are modelled with logistic regression.
P (ñ♂i) = e (ƍ+ƍi)/[1 + {e (ƍ+ƍi)}]
P (ñci) = e (γ+γi)/[1 + {e (γ+γi)}]
Parameters of logistic models (summarized in Table A1 and Table A2 of Appendix A) were used to infer number of emerged males and calling females between intervals to derive estimates of ᶘi. Because male bagworms typically die within one day after emergence [12], number of live adult males for any day i is equivalent to daily variation in abundance (♂i+1 − ♂i). Female bagworms are long-lived relative to males, but no tool is available to ‘age’ feral calling females at the time of sampling. The issue is circumvented by assuming that calling females are ‘young’ (<one day old) at the time of sampling (ñci = 0), with longevity (ȥ) set as either 1, 3, or 9 days. Under these conditions, ratios of males per calling female can be derived for any interval with the equations above.
ᶘ(0,ȥ) = (Ʃñ♂(ȥ) − ñ♂i=0)/ñi=0
Estimates of ci account for the relative abundance of males on any day i to derive mating probability of calling females (Equation (5)). Rules of thumb to infer the sex-ratio-dependent mating probability of calling females are as follows: ci = 0 when ᶘ(0,ȥ) < 0.5; ci = 0.25 when 0.5 < ᶘ(0,ȥ) < 1; ci = 0.5 when 1 ᶘ(0,ȥ) < 2; ci = 0.75 when 2 < ᶘȥ(0,ȥ), < 4; and ci = 1.0 when ᶘȥ(0,ȥ) > 4.
3. Results
3.1. General Trends
Proportion of live calling females (c/♀) was low in M. plana (5.0%), intermediate in O. kirbyi (12.3%), and high in T. ephemeraeformis (16.0%) (Table 1). Caution is warranted as to the interspecific rate of mating time-in due to systematically different sampling protocols in O. kirbyi and M. plana, as well as latitudinal clines in T. ephemeraeformis (see below).
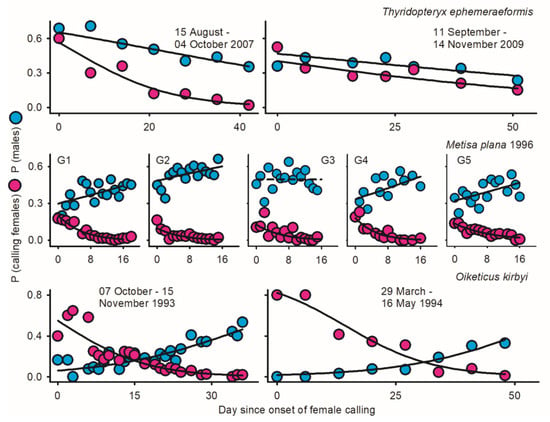
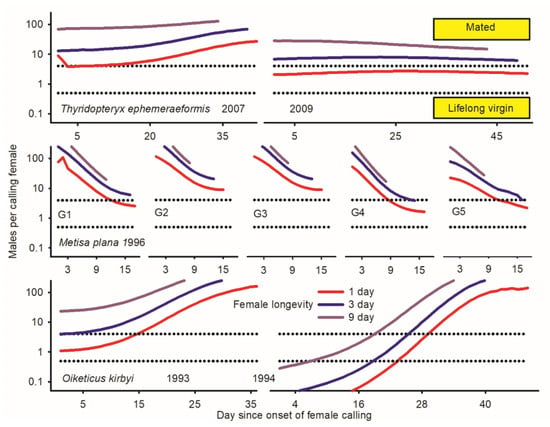
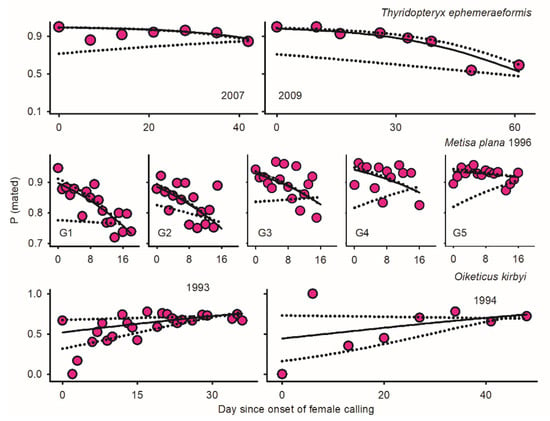
Protogyny in O. kirbyi and M. plana versus protandry in T. ephemeraeformis (Figure 1) predictably lead to decline/increment in relative abundance of males over time [P (♂i/Āi)] (Figure 2). The proportion of calling females significantly declined over time for all data sets (Figure 2)—as expected in populations with synchronous (non-overlapping) reproductive generations (see Discussion). With the exception of O. kirbyi in 1994, all calling females are expected to mate when adult longevity (ȥ) is ≥3 days (Figure 3). Mating success of time-out females declined over time for M. plana and T. ephemeraeformis, as opposed to an increase in mating probability over time in O. kirbyi (Figure 4).
Figure 2.
Temporal variation in proportions of males in adult populations [P (♂i/Āi), blue dots] and calling females [P (ci/♀i), pink dots] in three species of bagworms: Oiketicus kirbyi (1993–1994), Metisa plana during five consecutive generations in 1996 (G1 to G5), and Thyridopteryx ephemeraeformis in 2007 and 2009; data in 2008 are not depicted due to the short time series of abundance (14 days interval). Day since onset of female calling (set as day 0) was used as a time proxy in all analyses. Parameters of logistic regressions are as reported in Table A1 in Appendix A. Detailed sampling procedures and references are as shown in Figure 1.
Figure 3.
Temporal variation in ratios of males per calling females (ᶘ(0,ȥ) in Equation (9)) in three species of bagworms: Oiketicus kirbyi (1993–1994), Metisa plana during five consecutive generations in 1996 (G1 to G5), and Thyridopteryx ephemeraeformis in 2007 and 2009; data in 2008 are not depicted due to the short time series of abundance (14 days interval). Proportion of calling females that mate (ci, as in Equation (5)) was derived using ratios of males per calling females with variable longevity (ȥ = 1, 3, 9 days) as represented by horizontal dotted lines: (1) ci(ᶘ) = 0 when ᶘ(0,ȥ) < 0.5; (2) ci(ᶘ) = 0.25 when 0.5 < ᶘ(0,ȥ) < 1.0; (3) ci(ᶘ) = 0.50 when 1.0 < ᶘ(0,ȥ) < 2.0; (4) ci(ᶘ) = 0.75 when 2.0 < ᶘ(0,ȥ) < 4.0; and (5) ci(ᶘ) = 1 when ᶘ(0,ȥ) > 4.0. Day since onset of female calling (set as day 0) was used as a time proxy in all analyses. Parameters of logistic regressions are as reported in Table A1 in Appendix A. Detailed sampling procedures and references are as shown in Figure 1.
Figure 4.
Temporal variation of mating probability among time-out females (Equation (6)) in three species of bagworms: Oiketicus kirbyi (1993–1994), Metisa plana during five consecutive generations in 1996 (G1 to G5), and Thyridopteryx ephemeraeformis in 2007 and 2009; data in 2008 are not depicted due to the short time series of abundance (14 days interval). The solid lines represent the proportion of time-out females that mated as adults; dotted lines represent low- and high-function boundaries assuming that either calling females never mate or always mate (Equations (8) and (9)). Day since onset of female calling (set as day 0) was used as a time proxy in all analyses. Parameters of logistic regressions are reported in Table A1 in Appendix A. Detailed sampling procedures and references are as shown in Figure 1.
3.2. Oiketicus kirbyi
Adult females outnumbered males by a factor of ca 3.0 in 1993 and 1994 (Table 1). The extent of protogyny (interval between median date of female and male emergence) exceeded two weeks each year (Figure 1). More than two thirds of females were sampled as live calling at the onset of emergence, in part due to the low abundance of males; the proportion of calling females remained above 25% for about two weeks (Figure 3). Mating probability of time-out females increased over time (Figure 4) and ranged between 67.4 and 68.3% on a per year basis (Table 1).
In 1993, calling females were all expected to mate irrespective of time if they lived at least three days; in contrast, mating probability of short-lived females (one day) increased from 50 to 100% during the first 15 days of sampling and remained above 100% thereafter (Figure 3). Overall (season-long) mating probability of calling females increases with longevity from 77.1% (103.3/134) for a one-day lifespan to 100% for a lifespan > 3 days (Figure 3)
Under assumptions that calling females survive either one or three days in 1994, null (zero) mating success is expected during the first 24/18 days of sampling. Overall mating probability of calling females increases with longevity from 38.3% (34.5/90) for a one-day lifespan to 66.1% for a three-day lifespan and 84.4% for a nine-day lifespan (Figure 3).
3.3. Metisa plana
Depending upon generation G, females outnumbered males (G1, G4, and G5) or were outnumbered by males (G2 and G3); overall, the proportion of males averaged 45.2% of individuals (6630 ♂, 8046 ♀) (Table 1). Due to protogyny, the proportion of males relative to females significantly increased over time during four of five generations (Figure 2). The extent of protogyny, defined as the interval corresponding to 85% adult emergence for males and females, averaged 4.7 days on a per generation basis (Figure 1). The proportion of live calling virgins declined from ca 20% at the onset of sampling to <2% at the end of reproductive season, averaging 5.1% on a generation basis (Figure 2). The mating probability of time-out females declined over time (Figure 4) and ranged between 80.7 and 92.7% for different generations (Table 1).
Ratios of males per calling female generally exceeded 4:1 (Figure 3), implying that most calling females mated during their lifetime [estimates of 100% for lifespan > 3 days in all generations]. Even when assuming short (one day) longevity, more than 96% of calling females were expected to mate during each generation (Figure 3).
3.4. Oiketicus kirbyi Versus Metisa plana
Sampling protocols for O. kirbyi and M. plana fundamentally differed. Adults were sampled during the entire emergence cycle for O. kirbyi, as opposed to the late portion of emergence in M. plana (>50% emerged males and 85% emerged females) (Figure 1 and Figure 2). Comparison between species was standardized in O. kirbyi by using only late season estimates corresponding to >85% female emergence (21 and 42 days after onset of sampling in 1993 and 1994, respectively; Figure 1). Under this scenario, female M. plana were more than twice as likely to be sampled as live calling females than in O. kirbyi [M. plana: 405 of 8046 females, or 5.1%; O. kirbyi: 47 of 2216 females, or 2.1%].
3.5. Thyridopteryx ephemeraeformis in 2007–2009: Data Pooled by Year
Males were outnumbered by females each year, representing 35.1 to 43.2% of adults (Table 1). The extent of protandry (interval between median date of male and female emergence) lasted 3.8 days in 2007, <1 day in 2008, and 3.3 days in 2009 (Figure 1). On a per site basis, however, all patterns of emergence were observed: early, synchronous, and late emergence of males relative to females [56].
The proportions of males and calling females declined over time each year (Figure 2). The proportion of calling females was low in 2007 (6.6%), intermediate in 2008 (16.4%), and high in 2009 (23.7%) (Table 1). Mating probability of time-out females was high in 2007 (85.3%) and 2008 (87.5%), but low in 2009 (72.1%) (Table 1). Based on relative abundance of males, all calling females in 2007 are expected to mate (Figure 3). When data were pooled across latitudes in 2009, mating success of calling females with a one-day lifespan varied within a narrow range around 75% during the entire reproductive season; all females were expected to mate when longevity exceeded 3 days (Figure 3).
3.6. Thyridopteryx ephemeraeformis in 2007
Trends observed in 2007 cannot be extrapolated to any other year because bagworms were collected on a narrow geographic range (50 km radius around Lafayette in Indiana), as opposed to a large spatial range in 2008–2009 (including populations at southern and northern latitude that exhibit a very low/high incidence of female lifelong virginity [22,40]). As an example, data collected in Indiana at one site 120 km north of Lafayette (Hamlet: 41.28° N, 86.58° W) in late October 2007 at the end of the reproductive season (no calling females, only time-out females) revealed a low female mating probability (1079 of 1854 individuals, or 58.2% [57]) compared to 85.3% for mated females sampled between 40.0 and 40.5° N (Table 1).
3.7. Thyridopteryx ephemeraeformis in 2008
Based on the observation at Hamlet in 2007, a two-week haphazard experiment was conducted in 2008 including 118 sites sampled once between 3 and 16 October within a latitudinal range 39.56–41.28° N [40]. Logistic regression including two independent variables [day, latitude] revealed the following trends (Table 3). (1) The relative abundance of males increased with time and latitude. (2) Time-independent proportion of calling females increased with latitude. (3) Time-independent mating probability among time-out females declined with latitude (Table 4).
Table 4.
Effects of latitude/day of sampling (i/j) on three response variables (proportion of males among adults, proportion of calling females among adult females, and proportion of mated females among time-out females) for Thyridopteryx ephemeraeformis adults sampled in 2008; statistical effects of i/j were derived with logistic regression models. Unless otherwise specified (ns superscript), parameters were all statistically significant (p < 0.01). Day since onset of sampling (set as day 0) was used as a time proxy in all analyses.
3.8. Thyridopteryx ephemeraeformis in 2009
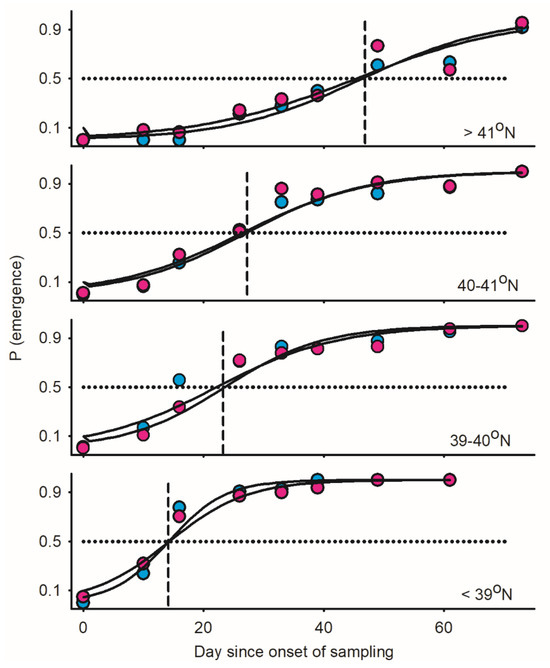
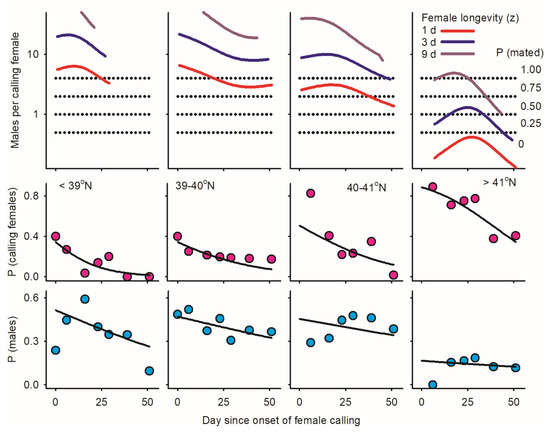
Data were divided into four latitudinal bands prior to analysis [<39°, 39–40° N, 40–41° N, >41° N]. Logistic regression models simultaneously factoring in day/sex/latitude revealed similar patterns of emergence for males and females (Wald ꭓ2 = 2.43, p = 0.1191) with steady increases in emergence over time (Wald ꭓ2 = 1563.71, 0.0001) and delayed emergence with increasing latitude (30 days difference between southernmost and northernmost latitudinal bands: Wald ꭓ2 = 485.48, p < 0.0001) (Figure 5). Both the proportions of males and calling females in adult populations decreased over time for all latitudinal bands (Figure 6). Most strikingly, proportion of calling females relative to time-out females increased from south to north; the same trend was observed, to a lower extent, for the proportion of males (Figure 6). When the trends above are combined, calling females are expected to mate at the following rates relative to latitude.
Figure 5.
Patterns of adult emergence [adult/(pupa + adult); blue and red dots for males and females] in Thyridopteryx ephemeraeformis populations sampled on ornamental trees in 2009 in the Midwest United States between North Tennessee and South Michigan (38.39–41.74° N (Figure 2 in [22]). Day since onset of emergence (day i = 0 at onset) was used as a proxy of time. Data were divided into four latitudinal bands for analysis. Parameters of logistic regression models are listed in Table A2 in Appendix A. Dotted and dashed lines represent dates corresponding to 50% adult emergence.
Figure 6.
Patterns of adult reproduction in Thyridopteryx ephemeraeformis populations sampled on ornamental trees in 2009 in the Midwest United States between North Tennessee and South Michigan (38.39–41.74° N; Figure 2 in [22]). Day since onset of sampling was used as a proxy of time, and data were divided into four latitudinal bands for analysis. Lower plots: proportion of males in adult populations [P (♂i/Āi), blue dots]. Middle plots: proportions of calling females among adults [P (ci/♀i), pink dots]. Upper plots: proportion of calling females that mate (ci, as in Equation (5)) as derived using ratios of males per calling females with variable longevity (ȥ = 1, 3, 9 days) as represented by horizontal dotted lines: (1) ci(ᶘ) = 0 when ᶘ(0,ȥ) < 0.5; (2) ci(ᶘ) = 0.25 when 0.5 < ᶘ(0,ȥ) < 1.0; (3) ci(ᶘ) = 0.50 when 1.0 < ᶘ(0,ȥ) < 2.0; (4) ci(ᶘ) = 0.75 when 2.0 < ᶘ(0,ȥ) < 4.0; and (5) ci(ᶘ) = 1 when ᶘ(0,ȥ) > 4.0. Parameters of logistic regression models are listed in Table A2 in Appendix A.
- (1)
- Assuming that longevity of females is equal to or exceeds 3 days, ratios of males per calling female (ᶘ) exceeded 4.00 for any day in the three southernmost latitudinal bands (<41° N), implying that all calling females mated as adults.
- (2)
- Assuming that females live for one day or less, the probability that calling females mate as adults declines with latitude for the three southernmost bands [92.4% at <39° N, 86.7% between 39 and 40° N; and 70.1% between 40 and 41° N].
- (3)
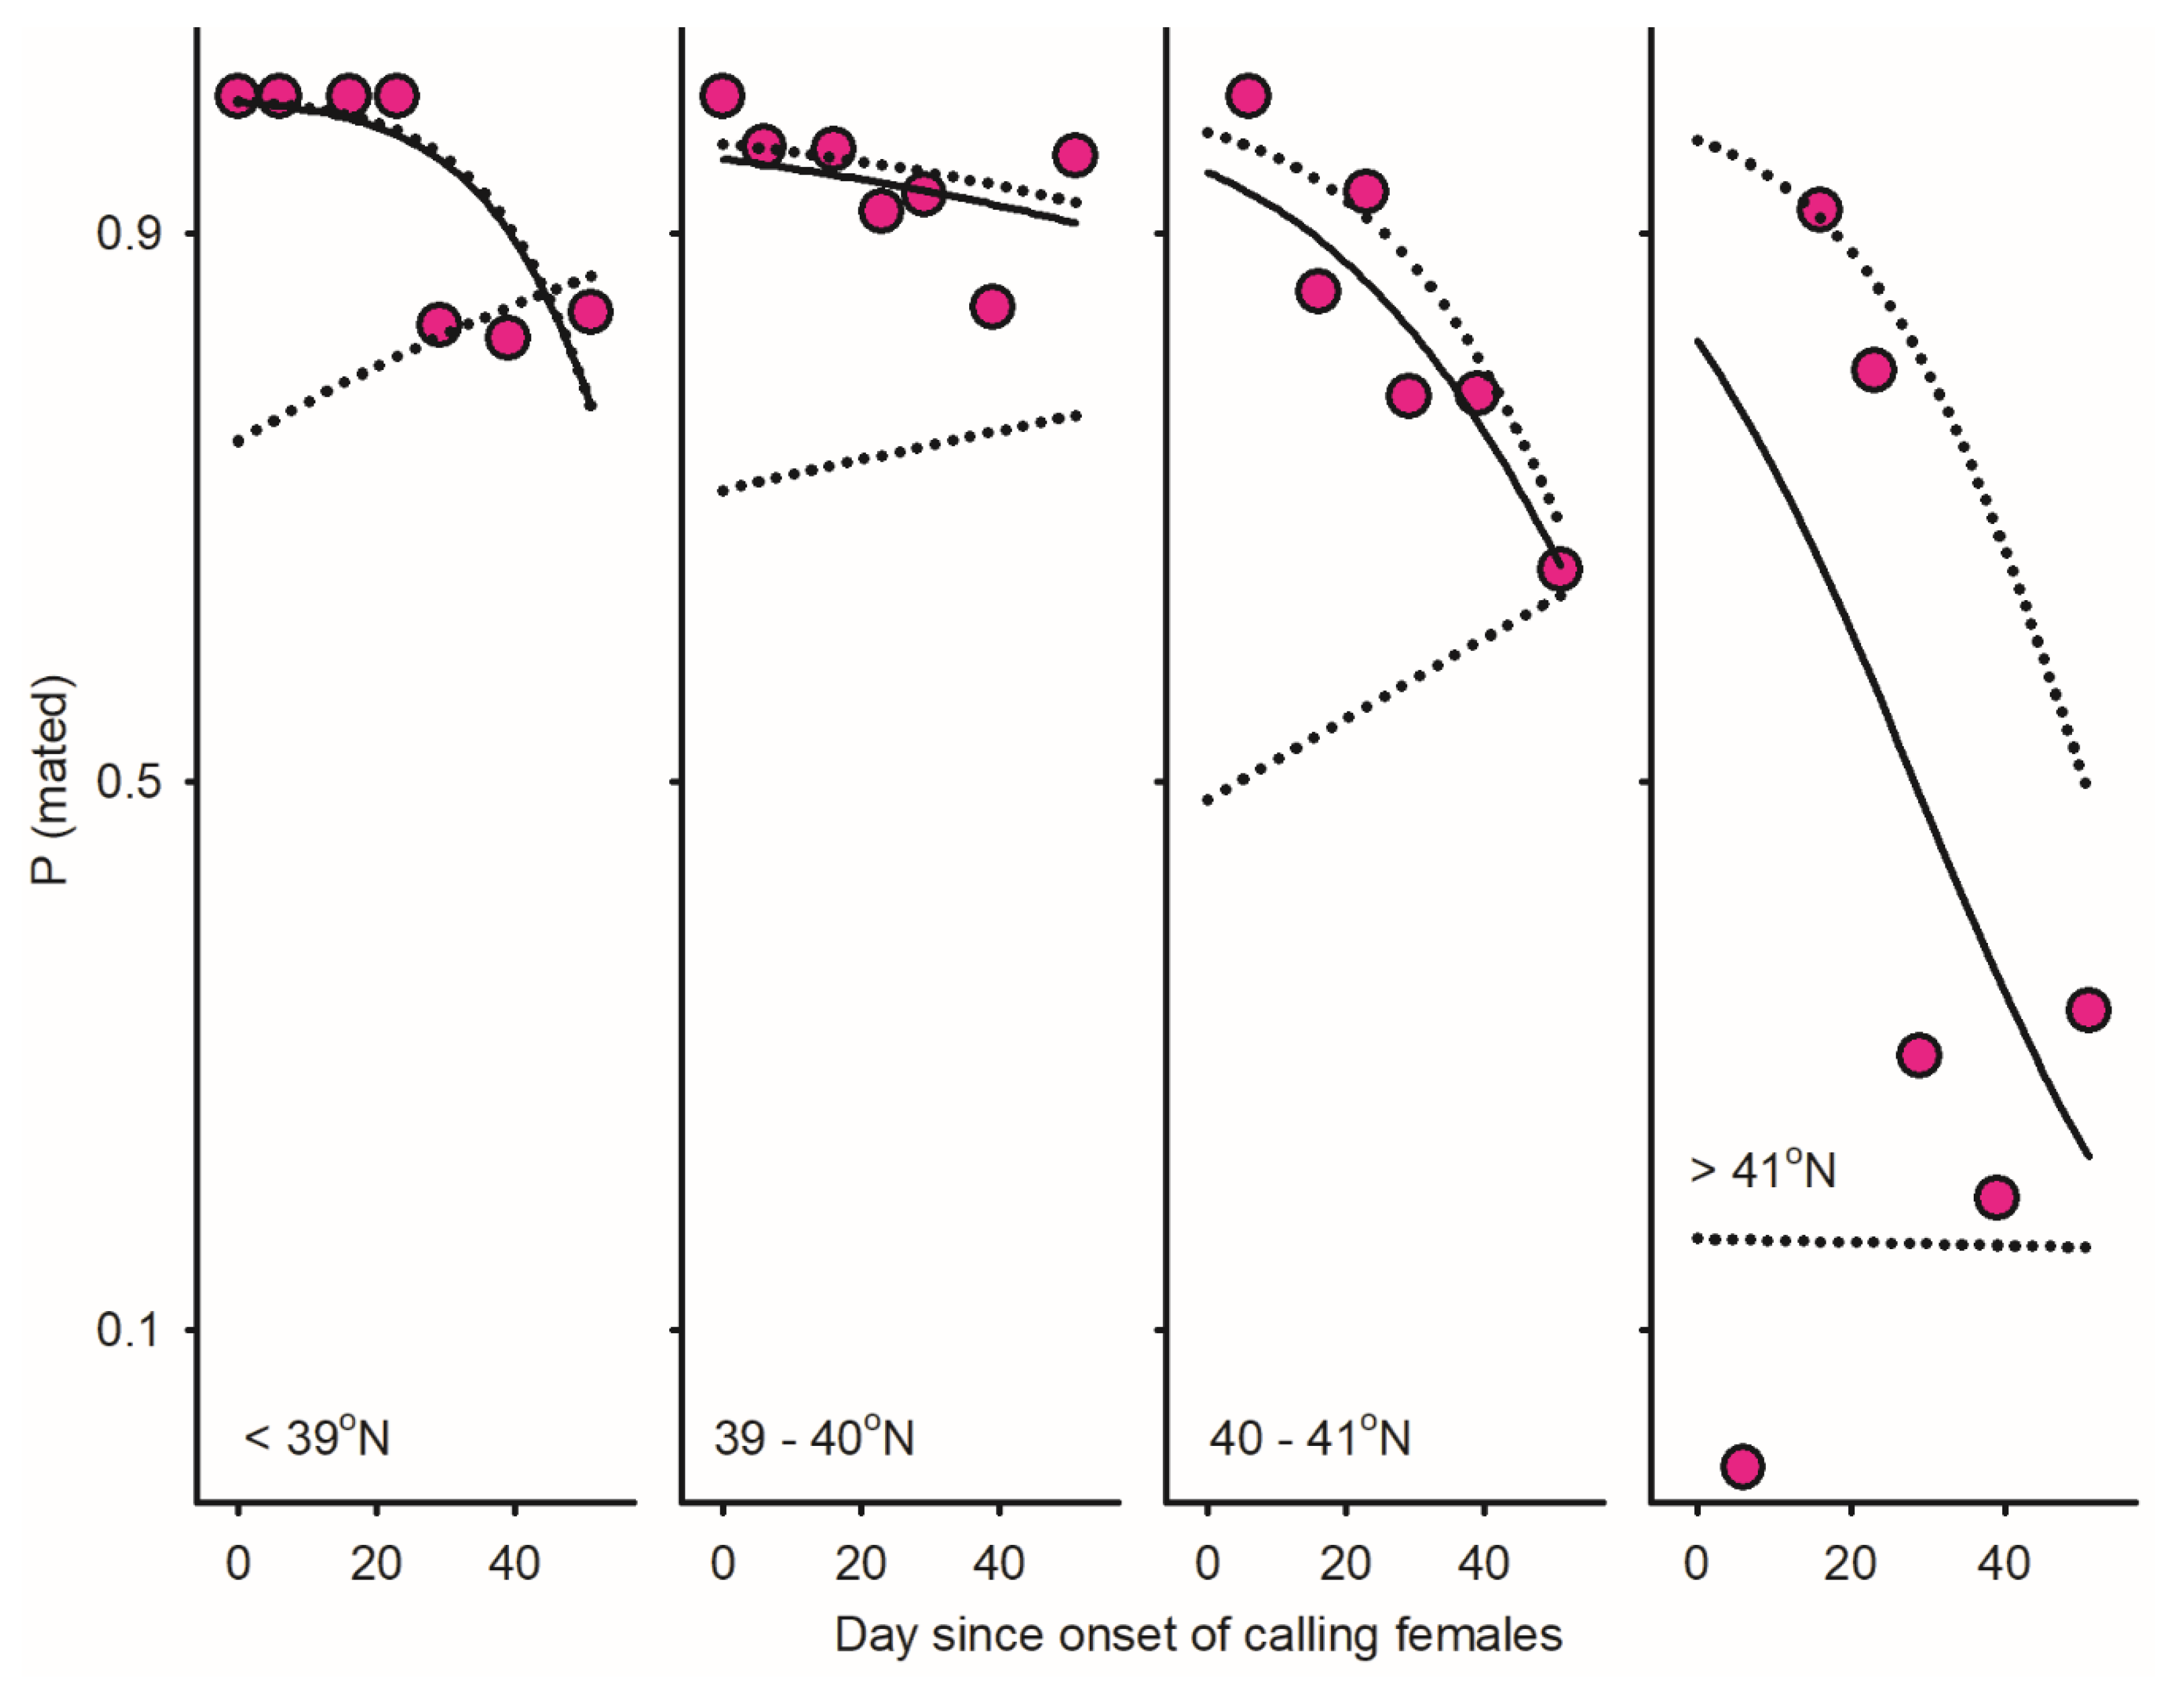
- Mating probability was lowest at latitudes >41° N (N = 173 calling females) and increased with female longevity (ȥ) from 0% when ȥ = 1, 34.2% when ȥ = 3, and 73.7% when ȥ = 9 (Figure 6 and Figure 7).Figure 7. Temporal variation in mating probability among time-out females (Equation (6)) in Thyridopteryx ephemeraeformis populations sampled on ornamental trees in 2009 in the Midwest United States between North Tennessee and South Michigan (38.39–41.74° N; Figure 2 in [22]). Day since onset of sampling was used as a proxy of time, and data were divided into four latitudinal bands for analysis. The solid lines represent the observed proportion of mated females; dotted lines represent low- and high-function boundaries assuming that either calling females never mate or always mate (Equations (8) and (9)). Parameters of logistic regression models are listed in Table A2 in Appendix A.
4. Discussion
In organisms with obligatory sexual reproduction, females are born virgin and need to access male sperm to produce viable offspring. This problem is simplified in holometabolous insects with complete metamorphosis because food acquisition and sexual activities are segregated into separate life history phases (transition between larval, pupal, and adult stages) [58,59,60]. Sessile female bagworms (Lepidoptera: Psychidae) reproduce within a self-constructed bag, thus providing a model system to parameterize the incidence of live ‘pheromone-calling’ females relative to time-out females. The low mating success of calling females is associated with extreme protogyny (early season male shortage; O. kirbyi in 1994) or late adult emergence in populations at the edge of the distribution range (T. ephemeraeformis at latitudes >41° N in 2019). Parameter estimates related to the reproductive status of females and sex ratio among adults, as derived here for Psychidae, could in theory be applied to three other taxonomic groups with common female monandry/flightlessness/neoteny: fireflies (Coleoptera: Lampyridae), twisted wings parasites (Strepsiptera), and scale insects (Hemiptera: Pseudococcidae) [12,17,61,62,63,64].
The definition of female mating time-in as developed in this study is nearly equivalent to live virginity, notwithstanding the passive emission of pheromone in bagworms [30,31]. Surveys of feral Lepidoptera captured with sweep nets or light traps often include punctual female mating success at the time of sampling (presence/absence of spermatophore or mating plug in the reproductive tract of females [10,65,66]. While these data are similar analytically to the incidence of mating time-in/time-out in female bagworms, future mating probability of live virgins is deemed unknowable in the absence of repeated measurements of abundance over time (including males, virgin females, and mated females). Data collected in female spruce budworms, Choristoneura fumiferana Clemens (Lepidoptera: Tortricidae), provide a system to link punctual virginity (based on proportion of mated females along age classes: young females foraging on host trees and mid-aged in-flight females captured at traps) and lifelong virginity (dead females collected on drop trays) [67,68,69,70].
Synchronous larval development in most bagworm species (including O. kirbyi, M. plana, T. ephemeraeformis; Table 1) leads to discrete (non-overlapping) reproductive generations, with males and females all emerging within a predetermined period. Considering monotonic trends of emergence patterns in discrete generations, the incidence of live calling females was higher at the onset of emergence (‘young’ females) than in the late season (when samples include mostly time-out females that previously mated or died as lifelong virgins). This mechanistic effect may be magnified in protogynous populations (early season female-biased sex ratio) relative to protandrous populations (early season male-biased sex ratio)—although similar trends were observed for protogynous O. kirbyi/M. plana and protandrous T. ephemeraeformis in this study. A moderate level of protandry is expected to increase the mating success of females/reduce the probability that live females are sampled while pheromone calling [56]. As hypothesized, negative effects of reproductive isolation on the mating success of protogynous female bagworms are buffered by a long lifespan [71,72]. From an applied perspective, populations of adult female T. ephemeraeformis can be managed with mating disruption using synthetic sex pheromone [28,29]. As in this study, the efficacy of mating disruption was assessed by recording numbers of live pheromone-calling ♀ (c), time-out mated ♀ (mŦ), and lifelong virgin ♀ (vŦ) females. Trees treated with pheromone consistently suppressed mating success among time-out females (40 of 310 females, or 12.9%) relative to control trees (254 of 308 females, 82.5%) (Table 1 in [28]). Re-invasion of treated plots by mated gravid females generally limits the feasibility of pheromone-based management in moths [73,74,75,76]; the issue is irrelevant in bagworms with sessile (non-dispersing) females.
Management of adult female M. plana in oil palm plantations may be achieved by mass trapping males with sticky traps each baited with two live calling females (thirty 60 × 30 cm traps/0.7 ha) [77]. Efficacy of mass trapping was assessed by recording the number of bags with eggs relative to the total number of female bags dissected (mŦ/♀); mass trapping reduced ‘mating probability’ of females from 35.7% (322 of 903 bags) to 20.3% (172 of 848 bags) (Table 1 in [77]). In addition to c, mŦ, and vŦ, the denominator may (or may not) have included female pupae (dead or alive) and females from past generations. More critically, the mass trapping experimental design may be fatally flawed as the control plots did not include sticky traps without calling females. It is conceivable that males were attracted to the large white surface of sticky traps per se, especially considering the large surface involved (7.7 m2/ha) (Figure 1 in [77]).
In principle, implementation of pheromone-based mating disruption/mass trapping requires a phenological model of adult emergence or monitoring tools to infer timing of emergence [78,79,80]. Other than the data provided here (Table 1), however, few studies report the phenology of bagworm reproduction in field conditions [81,82,83]. The paucity of data is surprising considering the ease of such measurements (relative to other insects) and the severe pest status of bagworms worldwide ([84], Table 4 in [85], Table 1 in [86], Table 1 in [87], Figure 2 in [88]).
Funding
This research received no external funding.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Acknowledgments
I wish to thank all my collaborators in Costa Rica, Indonesia, Malaysia, and U.S.A.
Conflicts of Interest
The author declares no conflicts of interest.
Appendix A
Note to Figure 1. Note [The proportion of emergence could in theory be used to infer variation in number of adults (A) relative to pupae (P) combined with sex-specific survival during the pupal stage (S) for males [P (♂i) = s♂ P (♂a/{♂p + ♂a}i)] and females [P (♀i) = s♀ P (♀a/{♀p + ♀a}i)]. Estimates of s♂ and s♀ are difficult to infer among species, even more so when they vary over time. For those reasons, individuals in the pupal stage were discarded from analysis. Functions of emergence above assume that s is equal to 1 (100% PUPAL survival) for both males and females].
Table A1.
Parameters of logistic regression models describing emergence patterns of males and females (Figure 1), proportions of males and calling females in adult populations (Figure 2), mating probability of time-out females (Equation (6) in text), and cumulative abundance of adult males and calling females (Equations (8) and (9)) in text). Data sources for the three bagworm species under investigation (Oiketicus kirbyi: Ok; Metisa plana: Mp; Thyridopteryx ephemeraeformis: Te) as summarized in Table 1 and Table 2. Unless specified (ns), all logistic regressions were statistically significant.
Table A2.
Parameters of logistic regression models describing demography of Thyridopteryx ephemeraeformis along four latitudinal bands in 2009: emergence patterns of males and females (Figure 5); proportions of males and calling females in adult populations (Figure 6); mating probability of time-out females (Figure 7); and cumulative abundance of adult males and calling females (Equations (8) and (9) in text). Data sources are as summarized in Table 1 and Table 2. Unless specified (ns), all logistic regressions were statistically significant.
References
- De Pasqual, C.; Groot, A.; Mappes, J.; Burfield-Steel, E. Evolutionary importance of intraspecific variation in sex pheromones. Trends Ecol. Evol. 2021, 36, 848–859. [Google Scholar] [CrossRef] [Scilit]
- Rizvi, S.A.H.; George, J.; Reddy, G.V.P.; Zeng, X.; Guerrero, A. Latest Developments in Insect Sex Pheromone Research and Its Application in Agricultural Pest Management. Insects 2021, 12, 484. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vickers, N.J. Animal communication: When I’m calling you, will you answer too? Curr. Biol. 2017, 27, R713–R715. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ahnesjö, I.; Kvarnemo, C.; Merilaita, S. Using potential reproductive rates to predict mating competition among individuals qualified to mate. Behav. Ecol. 2001, 12, 397–401. [Google Scholar] [CrossRef] [Scilit]
- Clutton-Brock, T.H.; Parker, G.A. Potential reproductive rates and the operation of sex selection. Q. Rev. Biol. 1992, 67, 437–456. [Google Scholar] [CrossRef] [Scilit]
- Kokko, H.; Wong, M. What determines sex roles in mate searching? Evolution 2007, 61–65, 1162–1175. [Google Scholar] [CrossRef] [Scilit]
- Lim, H.; Greenfield, M.D. Female arctiid moths, Utetheisa ornatrix, orient towards and join pheromonal choruses. Anim. Behav. 2008, 75, 673–680. [Google Scholar] [CrossRef] [Scilit]
- Parker, G.; Simmons, L.W. Parental investment and the control of sexual selection: Predicting the direction of sexual competition. Proc. R. Soc. B 1996, 263, 315–321. [Google Scholar] [CrossRef] [Scilit]
- Wiklund, C.; Kaitala, A.; Wedell, N. Decoupling of reproductive rates and parental expenditure in a polyandrous butterfly. Behav. Ecol. 1998, 9, 20–25. [Google Scholar] [CrossRef] [Scilit]
- Calabrese, J.M.; Ries, L.; Matter, S.F.; Debinski, D.M.; Auckland, J.N.; Roland, J.; Fagan, W.F. Reproductive asynchrony in natural butterfly populations and its consequences for female matelessness. J. Anim. Ecol. 2008, 77, 746–756. [Google Scholar] [CrossRef] [Scilit]
- Jocqué, R. Spider templates, sexual selection, and the risk of zerogamy: A taxonomist’s view. Beitraege Zur Araneol. 2025, 18, 124–160. [Google Scholar]
- Rhainds, M. Ecology of mating failure / lifelong virginity: A review of causal mechanisms in insects and arachnids. Entomol. Exp. Appl. 2019, 167, 73–84. [Google Scholar] [CrossRef] [Scilit]
- Stepien, T.L.; Zmurchok, C.; Hengenius, J.B.; Caja Rivera, R.M.; D’Orsogna, M.R.; Lindsay, A.E. Moth mating: Modeling female pheromone calling and male navigational strategies to optimize reproductive success. Appl. Sci. 2020, 10, 6543. [Google Scholar] [CrossRef] [Scilit]
- Umbers, K.D.L.; Symonds, M.R.E.; Kokko, H. The mothematics of female pheromone signalling: Strategies for aging virgins. Am. Nat. 2015, 185, 417–432. [Google Scholar] [CrossRef] [Scilit]
- Henshaw, J.M. Finding the one: Optimal choosiness under sequential mate choice. J. Evol. Biol. 2018, 31, 1193–1203. [Google Scholar] [CrossRef] [Scilit]
- Priklopil, T.; Kisdi, E.; Gyllenberg, M. Evolutionary stable mating decision for sequentially searching females and the stability of reproductive isolation by assertive mating. Evolution 2015, 69, 1015–1026. [Google Scholar] [CrossRef] [Scilit]
- Cock, R.D.; Faust, L.; Lewis, S. Courtship and Mating in Phausis reticulata (Coleoptera: Lampyridae): Male Flight Behaviors, Female Glow Displays, and Male Attraction to Light Traps. Fla. Entomol. 2014, 97, 1290–1307. [Google Scholar] [CrossRef] [Scilit]
- Janetos, A.C. Strategies of mate choice: A theoretical analysis. Behav. Ecol. Sociobiol. 1980, 7, 107–122. [Google Scholar] [CrossRef] [Scilit]
- Johnson, T.L.; Elgar, M.A.; Symonds, M.R.E. Movement and olfactory signals: Sexually dimorphic antennae and female flightlessness in moth. Front. Ecol. Evol. 2022, 10, 919093. [Google Scholar] [CrossRef] [Scilit]
- Wittenberg, J.F.; Tilson, R.L. The evolution of monogamy: Hypotheses and evidence. Annu. Rev. Ecol. Syst. 1980, 11, 197–232. [Google Scholar] [CrossRef] [Scilit]
- Cushman, J.H.; Boggs, C.L.; Weiss, S.B.; Murphy, D.D.; Harvey, A.W.; Ehrlich, P.R. Estimating female reproductive success of a threatened butterfly: Influence of emergence time and host plant phenology. Oecologia 1994, 99, 194–200. [Google Scholar] [CrossRef] [Scilit]
- Lynch, H.J.; Rhainds, M.; Calabrese, J.M.; Cantrell, S.; Cosner, C.; Fagan, W.F. How climate extremes—Not means—Define a species’ geographic range boundary via a demographic tipping point. Ecol. Monogr. 2014, 84, 131–149. [Google Scholar] [CrossRef] [Scilit]
- Rosenheim, J.A.; Jepsen, S.J.; Matthews, C.E.; Smith, D.S.; Rosenheim, M.R. Time limitation, egg limitation, the cost of oviposition, and lifetime reproduction by an insect in nature. Am. Nat. 2008, 172, 486–496. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Elzinga, J.A.; Chevasco, V.; Grapputo, A.; Mappes, J. Influence of male mating history on female reproductive success among monandrous Naryciinae (Lepidoptera: Psychidae). Ecol. Entomol. 2011, 36, 170–180. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M.; Leather, S.R.; Sadof, C.S. Polyphagy, flightlessness, and reproductive output of females: A case study with bagworms (Lepidoptera: Psychidae). Ecol. Entomol. 2008, 33, 663–672. [Google Scholar] [CrossRef] [Scilit]
- Stephens, C.S. Oiketicus kirbyi (Lepidoptera: Psychidae): A pest of bananas in Costa Rica. J. Econ. Entomol. 1962, 55, 381–386. [Google Scholar] [CrossRef] [Scilit]
- Neal, J.W. Significance of opposing abdominal tergal spines on the pupae of the bagworm Thyridopteryx ephemeraeformis (Lepidoptera: Psychidae). J. Kans. Entomol. Soc. 1982, 55, 605–616. [Google Scholar]
- Klun, J.A.; Neal, J.W.; Leonhardt, L.; Schwarz, M. Suppression of female bagworm, Thyridopteryx ephemeraeformis reproduction potential with its sex pheromone, 1-methylbutyl decanoate. Entomol. Exp. Appl. 1986, 40, 231–238. [Google Scholar] [CrossRef] [Scilit]
- Leonhardt, B.A.; Neal, J.W.; Klun, J.A.; Schwarz, M.; Plimmer, J.R. An unusual lepidopteran sex pheromone system in the bagworm moth. Science 1983, 219, 314–316. [Google Scholar] [CrossRef] [Scilit]
- Abdullah, F.A.; Sabri, M.S.M.; Sina, I.; Fauzee, F.; Isa, S.M. Response of the male bagworm moth (Metisa plana Walker, Lepidoptera Psychidae) toward female bagworm pheromone lure in wind tunnel bioassays. Asia Life Sci. 2012, 21, 375–389. [Google Scholar]
- Rhainds, M. Natural mating disruption in a protogynous bagworm (Lepidoptera: Psychidae). Ecol. Entomol. 2018, 43, 543–546. [Google Scholar] [CrossRef] [Scilit]
- Kaufmann, T. Dicymolomia julianalis (Lepidoptera: Pyralidae) as an endoparasite of the bagworm, Thyridopteryx ephemeraeformis (Psychidae): Its relation to host, life history and gonad development. Pan-Pac. Entomol. 1985, 61, 200–209. [Google Scholar]
- Sheppard, R.F. The bagworm, Thyridopteryx ephemeraeformis: A model system for studying the principles of population dynamics. Bull. Entomol. Soc. Am. 1975, 21, 153–156. [Google Scholar] [CrossRef] [Scilit]
- Davis, D.R. Bagworm Moths of the Western Hemisphere; United States National Museum Bulletin: Washington, DC, USA, 1964; Volume 244, pp. 1–233. [Google Scholar]
- Jones, F.M. The mating of the Psychidae. Trans. Ann. Entomol. Soc. 1927, 53, 293–312. [Google Scholar]
- Syed, R.A. Bionomics of the three important species of bagworms on oil palm. Malays. Agric. J. 1978, 51, 392–398. [Google Scholar]
- Thangavelu, S.; Gunasekaran, K. Aspects of mating behavior in bagworm moth Clania cramerii (Westwood). Entomon 1982, 7, 457–462. [Google Scholar]
- Rhainds, M.; Gries, G.; Chinchilla, C.M. Pupation site and emergence time influence the mating success of bagworm females, Oiketicus kirbyi. Entomol. Exp. Appl. 1995, 77, 183–187. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M.; Gries, G.; Min, M.M. Size- and density-dependent reproductive success of bagworms, Metisa plana. Ent. Exp. Appl. 1999, 91, 375–383. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M. Spatio-temporal variation in mating success of female bagworms. Entomol. Exp. Appl. 2013, 146, 123–129. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M.; Gries, G.; Saleh, A. Density and pupation site in of apterous female bagworms, Metisa plana (Lepidoptera: Psychidae), influence the distribution of emergent larvae. Can. Entomol. 1998, 130, 603–613. [Google Scholar] [CrossRef] [Scilit]
- Hardenberg, C.B. South African Bagworms: Their Transformations, Life-History, and Economic Importance. Part II. Ann. Natal Mus. 1919, 4, 143–227. [Google Scholar]
- Haseman, L. The evergreen bagworms. Mo. Agric. Exp. Stn. Bull. 1912, 104, 309–330. [Google Scholar]
- Thangavelu, S.; Ravindranath, M.H. Morphology and life-history of the bag-worm moth Clania cramerii (Westwood). J. Nat. Hist. 1985, 19, 1–19. [Google Scholar] [CrossRef] [Scilit]
- Crutwell, R.E. The bagworms (Lep: Psychidae) of Trinidad and their natural enemies. Tech. Bull. Commonw. Inst. Biol. Control 1974, 17, 127–159. [Google Scholar]
- Gara, R.I.; Sarango, A.; Cannon, P.G. Defoliation of an Ecuadorian mangrove forest by the bagworm Oiketicus kirbyi (Lepidoptera: Psychidae). J. Trop. For. Sci. 1990, 3, 181–186. [Google Scholar]
- Basri, M.W. Life History, Ecology and Economic Impact of the Bagworm, Metisa plana Walker (Lepidoptera: Psychidae) on the Oil Palm, Elaeis guineensis Jacquin (Palmae), in Malaysia. Ph.D. Thesis, University of Guelph, Guelph, ON, Canada, 1993; p. 217. [Google Scholar]
- Kamarudin, N.H.J.; Basri, M.W.; Robinson, G.S. Common bagworm pests (Lepidoptera: Psychidae) of oil palm in Malaysa with notes to related Southeast Asian species. Malay. Nat. J. 1994, 48, 93–123. [Google Scholar]
- Barrows, E.M. Some factors affecting population size of the bagworm, Thyridopteryx ephemeraeformis (Lepidoptera: Psychidae). Environ. Entomol. 1974, 3, 929–932. [Google Scholar] [CrossRef] [Scilit]
- Cox, D.L.; Potter, D.A. Within-crown distribution of male and female bagworm (Lepidoptera: Psychidae) pupae on juniper as affected by host defoliation. Can. Entomol. 1988, 120, 559–567. [Google Scholar] [CrossRef] [Scilit]
- Cronin, J.T.; Gill, D.E. The influence of host distribution, sex, and size on the level of parasitism by Itoplectis conquisitor (Hymenoptera: Ichneumonidae). Ecol. Entomol. 1989, 14, 163–173. [Google Scholar] [CrossRef] [Scilit]
- Kaufmann, T. Observations on the biology and behavior of the evergreen bagworm moth, Thyridopteryx ephemeraeformis (Lepidoptera: Psychidae). Ann. Entomol. Soc. Am. 1968, 61, 38–44. [Google Scholar] [CrossRef] [Scilit]
- Johnson, M.P.; Potter, D.A.; Gilmore, G.S. Suitability of juniper cultivars for survival and growth of the bagworm. J. Environ. Hortic. 1993, 11, 167–170. [Google Scholar] [CrossRef] [Scilit]
- Lemke, H.D.; Raupp, M.J.; Shrewsbury, P.M. Efficacy and costs associated with the manual removal of bagworms, Thyridopteryx ephemeraeformis, from Leyland cypress. J. Environ. Hortic. 2005, 23, 123–126. [Google Scholar] [CrossRef] [Scilit]
- Rivers, D.B.; Antonelli, A.L.; Yoder, J.A. Bags of the Bagworm Thyridopteryx ephemeraeformis (Lepidoptera: Psychidae) Protect Diapausing Eggs from Water Loss and Chilling Injury. Ann. Entomol. Soc. Am. 2002, 95, 481–486. [Google Scholar] [CrossRef] [Scilit]
- Larsen, E.; Calabrese, J.M.; Rhainds, M.; Fagan, W.F. How protandry and protogyny affect female mating failure: A spatial population model. Entomol. Exp. Appl. 2013, 146, 130–140. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M.; Sadof, C.S. Fitness consequence of pupation site for bagworms (Lepidoptera: Psychidae) on arborvitae. Ann. Appl. Entomol. Zool. 2009, 44, 323–329. [Google Scholar] [CrossRef] [Scilit]
- Manthey, C.; Metcalf, C.J.E.; Monaghan, M.T.; Steiner, U.K.; Roff, J. Rapid growth and the evolution of complete metamorphosis in insects. Proc. Natl. Acad. Sci. USA 2024, 38, e2402980121. [Google Scholar] [CrossRef] [Scilit]
- McMahon, D.P.; Hayward, A. Why grow up? A perspective on insect strategies to avoid metamorphosis. Ecol. Entomol. 2016, 41, 505–515. [Google Scholar] [CrossRef] [Scilit]
- Konopova, B. Evolution of insect metamorphosis—An update. Curr. Opin. Insect Sci. 2025, 67, 101289. [Google Scholar] [CrossRef] [Scilit]
- Baudry, G.; Hopkins, J.; Watts, P.C.; Kaitala, A. Female sexual signaling in a capital breeder, the European glow-worm Lampyris noctiluca. J. Insect Behav. 2021, 34, 16–25. [Google Scholar] [CrossRef] [Scilit]
- Kathirithamby, J.; Hrabar, M.; Delgado, J.A.; Collantes, F.; Dötterl, S.; Windsor, D.; Gries, G. We do not select, nor are we choosy: Reproductive biology of Strepsiptera (Insecta). Biol. J. Linn. Soc. 2015, 116, 221–228. [Google Scholar] [CrossRef] [Scilit]
- Normark, B.B. The evolution of alternative genetic systems in insects. Annu. Rev. Entomol. 2003, 48, 397–423. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Normark, B.B.; Johnson, N.A. Niche explosion. Genetica 2011, 139, 551–564. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Burns, J.M. Mating frequency in natural populations of skippers and butterflies as determined by spermatophore counts. Proc. Natl. Acad. Sci. USA 1968, 61, 852–859. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wiklund, C.; Forsberg, J. Sexual size dimorphism in relation to female polygamy and protandry in butterflies: A comparative study of Swedish Pieridae and Satyridae. Oikos 1991, 60, 373–381. [Google Scholar] [CrossRef] [Scilit]
- Greenbank, D.O.; Schaefer, G.W.; Rainey, R.C. Spruce budworm (Lepidoptera: Tortricidae) moth flight and dispersal: New understanding from canopy observations, radar, and aircraft. Mem. Entomol. Soc. Can. 1980, 110, 1–49. [Google Scholar] [CrossRef] [Scilit]
- Régnière, J.; Delisle, J.; Sturtevant, B.R.; Garcia, M.; Saint-Amant, R. Modeling migratory flight in the spruce budworm: Temperature constraints. Forests 2019, 10, 802. [Google Scholar] [CrossRef] [Scilit]
- Thomas, A.W.; Borland, S.A.; Greenbank, D.O. Field fecundity of the spruce budworm (Lepidoptera: Tortricidae) as determined from regression relationships between egg complement, fore wing length, and body weight. Can. J. Zool. 1980, 58, 1608–1611. [Google Scholar] [CrossRef] [Scilit]
- Rhainds, M.; Delisle, J.; Boulanger, Y.; Labrecque, A. Inverse size-dependent phenology of female spruce budworms along reproductive and behavioral classes: An empirical study. Entomol. Exp. Appl. 2022, 170, 612–622. [Google Scholar] [CrossRef] [Scilit]
- Degen, T.; Hovestadt, T.; Mittesser, O.; Hölker, F. High female survival promotes evolution of protogyny and sexual conflict. PLoS ONE 2015, 10, e0118354. [Google Scholar] [CrossRef] [Scilit]
- Degen, T.; Hovestadt, T.; Mittesser, O.; Hölker, F. Altered sex-specific mortality and female mating success: Ecological effects and evolutionary responses. Ecosphere 2017, 8, e10820. [Google Scholar] [CrossRef] [Scilit]
- Roscoe, L.E.; MacKinnon, W.; Régnière, J.; Forbes, G.; Brophy, M.; Lamb, R. Use of a sprayable sex pheromone formulation in landscape-level control of Choristoneura fumiferana populations. Insects 2022, 13, 1175. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wearing, C.H. Life table simulations of a univoltine codling moth, Cydia pomonella, population. 3. Impact of immigration on the effectiveness of mating disruption. Biocontrol Sci. Technol. 2022, 32, 1156–1176. [Google Scholar] [CrossRef] [Scilit]
- Curtiss, R.T.; Nottingham, L.; Adams, C.G.; Gut, L.J. Estimating plume reach and trapping radii for male and female Cydia pomonella (Lepidoptera: Tortricidae) captured in pheromone-kairomone baited traps in Washington State apple orchards under mating disruption. J. Econ. Entomol. 2023, 116, 1592–1603. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Campbell, J.F.; Miller, J.; Peterson, J.; Lingren, B. Evaluation of mating disruption for suppression of Plodia interpunctella populations in retail stores. Insects 2025, 16, 691. [Google Scholar] [CrossRef] [Scilit]
- Kamarudin, N.; Ahmad, S.N.; Arshad, O.; Whahid, M.B. Pheromone mass trapping of bagworm moths, Metisa plana Walker (Lepidoptera: Psychidae), for its control in mature oil palms in Perak, Malaysia. J. Asia-Pac. Entomol. 2010, 13, 101–106. [Google Scholar] [CrossRef] [Scilit]
- Ferracini, C.; Pogolotti, C.; Rama, F.; Lentini, G.; Saitta, V.; Mereghetti, P.; Mancardi, P.; Alma, A. Pheromone-mediated mating disruption as management opotion for Cydia spp. In chestnut orchard. Insects 2021, 12, 905. [Google Scholar] [CrossRef] [Scilit]
- Jones, V.P.; Wiman, N.G. Modeling the interaction of physiological time, seasonal weather patterns, and delayed mating on population dynamics of codling moth, Cydia pomonella (L.) (Lepidoptera: Tortricidae). Popul. Ecol. 2012, 54, 421–429. [Google Scholar] [CrossRef] [Scilit]
- Rincon, D.F.; Gutierrez-Illan Crowder, D.W. Assessing pest control treatments from phenology models and field data. Pest Manag. Sci. 2024, 81, 1851–1859. [Google Scholar] [CrossRef] [Scilit]
- Hardenberg, C.B. South African Bagworms: Their Transformations, Life-History, and Economic Importance. Part I. Ann. Natal Mus. 1917, 3, 619–686. [Google Scholar]
- Morden, R.D.; Waldbauer, G.P. The developmental rates of Thyridopteryx ephemeraeformis from four latitudes and notes on its biology (Lepidoptera: Psychidae). Entomol. News 1971, 82, 151–156. [Google Scholar]
- Morden, R.D.; Waldbauer, G.P. Seasonal and daily emergence patterns of adult Thyridopteryx ephemeraeformis (Lepidoptera: Psychidae). Entomol. News 1971, 82, 219–224. [Google Scholar]
- Entwistle, P.F. Observations on the biology of four species of Psychidae (Lepidoptera) on Theobroma cacao L. in Western Nigeria. Proc. R. Entomol. Soc. Lond. 1963, 38, 145–152. [Google Scholar] [CrossRef] [Scilit]
- Basri, M.W.; Hasan, A.H.; Masijan, Z. Bagworms (Lepidoptera: Psychidae) of oil palms in Malaysia. PORIM Occas. Pap. 1988, 23, 1–38. [Google Scholar]
- Rhainds, M.; Davis, D.R.; Price, P.W. Bionomics of bagworms (Lepidoptera: Psychidae). Annu. Rev. Entomol. 2009, 54, 209–226. [Google Scholar] [CrossRef] [Scilit]
- Induria, S.K.; Agrawal, A. First record of bagworm (Lepidoptera: Psychidae) Acanthopsyche (Pteroma) from Bastar Forest. Int. J. Technol. 2022, 12, 23–24. [Google Scholar] [CrossRef] [Scilit]
- Lelana, N.E.; Utami, S.; Darmawan, U.W.; Nuroniah, H.S.; Darwo Asmaliyah Haneda, N.F.; Arinana Darwiati, W.; Anggraeni, I. Bagworms in Indonesian plantation forests: Species composition, pest status, and factors that contribute to outbreaks. Diversity 2022, 14, 471. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2026 by the author. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license.