


Abstract
Rice is the most important crop for worldwide consumers. The water utilization of rice planting is more than 50% of agricultural water in China, and it is necessary to breed water-saving and drought-resistant rice. The rice variety Dianheyou 615 can be planted in the paddy and upland fields, which satisfies rice production farmers in mountainous regions of Yunnan. We aimed to explore the variations in Magnaporthe oryzae isolates collected from Dianheyou 615 planted in paddy or upland fields. Through pathogenicity tests, we found that most isolates had the highest pathogenicities, but there were no significant differences between the paddy and upland isolates. By a combination of monogenetic and elite rice lines, with a further resistance assessment, the monogenetic lines with Pi9, Diantun 506, and Lvhan 1 displayed better resistances. Moreover, we re-sequenced 15 isolates to explore their genetic variations. Our results showed that the source of the upland isolates may have been the offspring of the paddy isolates, but there were many genes with specifically found SNPs in two populations that would develop subdivisions after long-time planting. Overall, we compared the pathogenicities and genetic variations in blast isolates from the planting of Dianheyou 615 in paddy and upland fields, which provided references for the influence of the planting environment on population subdivisions.
1. Introduction
Rice is the staple food for over 50% of the global population. The yield potential of rice has been increasing since the breeding of semi-dwarf rice. In China, the successful breeding of hybrid rice and the launching of the super rice program greatly improved rice yield. However, paddy rice planting requires large amounts of water, which consume 50% of agricultural water in China [1]. The shortage of water is limiting rice development; thus, it is necessary to develop water-saving and drought-resistance rice, which would be great achievements for food security in China [2,3,4]. The rice variety Dianheyou 615 is widely used in the Yunnan area and can be planted both in paddy and upland areas. Moreover, the planting of this variety relies only on rainfall, which solves the problems of rice planting in the upland and mountainous districts of Yunnan.
Rice blast disease, caused by Magnaporthe oryzae (Hebert) Barr., threatens global rice production and food safety [5]. Populations of M. oryzae were widely distributed in rice planting regions, which provided global resources and the ability to exploit the genetic differentiation and evolution of M. oryzae [6]. Nowadays, the populations of M. oryzae are divided into four lineages; lineage one contains more genetic diversity and recombination isolates, while the other three lineages are non-admixed and clonal isolates [7]. Moreover, the effector number, rice subdivisions, and sexual deficits drive the formation of different lineages.
Both mountainous areas and periods of uneven rainfall limit crop production in Yunnan. The popularization of the rice variety Dianheyou 615 made it easier to plant rice in artificial irrigation-deficient areas. The Yunnan area, located in South East Asia, is regarded as the origin of M. oryzae’s diversity [8]. Here, we found rice blast disease in Dianheyou 615 crops whenever they were planted in paddy or upland areas. There was no result of the comparison of the pathogenicities and genetic variations in the blast populations in one rice variety planted in two different agricultural ecosystems. In order to explore the differences of M. oryzae collected from the planting of Dianheyou 615 in upland and paddy fields, we tested pathogenicities and sequenced 15 isolate genomes for further clarification of the variations between the isolates from different planting environments.
2. Materials and Methods
2.1. Collection of Rice Blast Isolates
In total, 22 M. oryzae isolates were collected from the leaves and panicles of rice planted in the regions of Yiliang, Jingdong, Linxiang, and Lincang, and two isolates were collected from the lesions on the Digitaria sanguinalis grass in Yiliang county (Table 1). The isolates were purified by single spore isolation and transferred onto filter paper for long-time conservation at −80 °C.
Table 1.
The information for collected M. oryzae isolates.
2.2. Rice Varieties
The LTH (Lijiangxintuanheigu) and monogenetic lines were given by Dr. Yo-shimichi Fukuta from the Japan International Research Center for Agricultural Sciences. The Diheyou 615, Diantun 502, and Diantun 506 were given by Dr. Dandan Li from the Rice Research Institute of Yunnan Agricultural University. The other rice varieties, including Lvhan 1, Linhan 1, Ridao 1, Danhandao 53, Luodao 998, Baohan 1, Zhenghan 10, and Yuanhandao 3, were bought from commercial companies.
2.3. Pathogenicity Test
The filter paper containing rice blast isolate was cultivated on the oatmeal agar medium under continuous lighting for sporulation. After 8-12 days, the spores were scraped by sterilized distilled water with 0.01% Tween 20, and the final concentration of spore suspension was adjusted to 1 × 10⁵ conidia/mL. The three seedlings of each rice variety were planted into one pot in a growth chamber. The 21-old-day seedlings were used to be inoculated by spore suspension spraying. The inoculated seedlings were incubated in a growth incubator with >80% humidity at 25 °C in the dark for 20–24 h and then transferred to the growth chamber for 6 days. The pathogenicity scores were evaluated at 7 days post inoculations according to Hayashi and Fukuta’s method [9,10]. The pathogenicity test was performed twice. , PF ≥ 70% is the highest pathogenicity, 50% ≤ PF < 70% is high pathogenicity, 20% ≤ PF < 50% is medium pathogenicity and PF < 20% is weak pathogenicity. .
2.4. Fungicide and Osmotic Stress-Inducer Treatment
The filter paper containing rice blast isolated was cultivated on complete medium (CM) for 7 days and transferred to new CM plates containing fungicide (0.1 mg/L ketoconazole, 0.1 mg/L azoxystrobin, and 1 mg/L tebuconazole), and osmotic stress-inducer (1 M KCl, 1 M NaCl, and 1.2 M sorbitol). After 7 days, the diameters of each colony were measured, and the inhibitory rates were calculated by the following equation: * means the diameter of the fungal disc.
2.5. Genome Sequencing
The blast-fungal samples were prepared according to the previous method. The CTAB (Cetyl Trimethyl Ammonium Bromide) method was used to extract the genome of the blast fungus. The whole genomes of 15 M. oryzae isolates were sequenced using Illumina NovaSeq PE150 at the Beijing Novogene Bioinformatics Technology Co., Ltd., Beijing, China. The sequenced reads were mapped to the reference genome (https://www.ncbi.nlm.nih.gov/assembly/GCF_000002495.2, accessed on 14 October 2011) using BWA software (V0.7.8). The sequencing data were deposited at Sequence Read Archive with PRJNA948861.
2.6. Single Nucleotide Polymorphism Analysis
SAMTOOLS was used for the detection of the individual SNP (single nucleotide polymorphism). The maximum-likelihood trees were constructed based on the SNP data, including 13 rice-infecting isolates sequenced in this study and a previously sequenced Setaria-infecting isolate SV9610 with default parameter values by FastTree v2.1.9 and displayed with Evolview. Frappe 12.10.0 was used for Structure analysis.
2.7. Statistical Analyses
Statistically significant differences were calculated by ANOVA Duncan’s test or Student t-test.
3. Results
3.1. Pathogenicity of M. oryzae Isolates from Paddy and Upland Fields
We obtained 24 isolates through single-spore isolation from 4 areas: Yiliang, Jingdong, Linxiang, and Lincang (Table 2). Among these isolates, 19 isolates were isolated from Dianheyou 615 (12 isolates from an upland field and 7 isolates from a paddy field), 3 isolates were isolated from local conventional upland rice in Lancang county, and 2 isolates were isolated from D. sanguinalis grass near a Dianheyou 615 planting upland field in Yiliang county. A total of 36 rice varieties, including 25 monogenetic lines harboring major resistant genes, 8 upland varieties, 2 paddy varieties and Dianheyou 615, were used for pathogenicity tests of the 24 isolates.
Table 2.
Pathogenicity frequency of M. oryzae.
The pathogenicity frequencies of the 24 test isolates ranged from 0.00% to 100.00% (Table 2). Pathogenicity frequencies of 17 isolates (YL22S1, YL22S2, YL22S3, YL22H1, YL22H2, YL22H3, YL22H5, YL22H7, YL22H9, JD22S1, JD22S2, LC22C3, LC22H1, LC22H2, LC22H3, LX22S1, and LX22S2) were over 70%. Five isolates (LC22C1, LC22C2, LX22H1, LX22H2, and LX22H3) with high pathogenicity were from Lancang and Linxiang. The two grass isolates (YL22M1 and YL22M2) showed no pathogenicity. These results showed that most test isolates with high pathogenicity were isolated from the four areas.
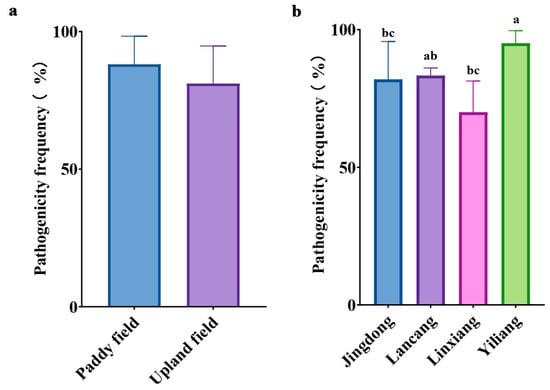
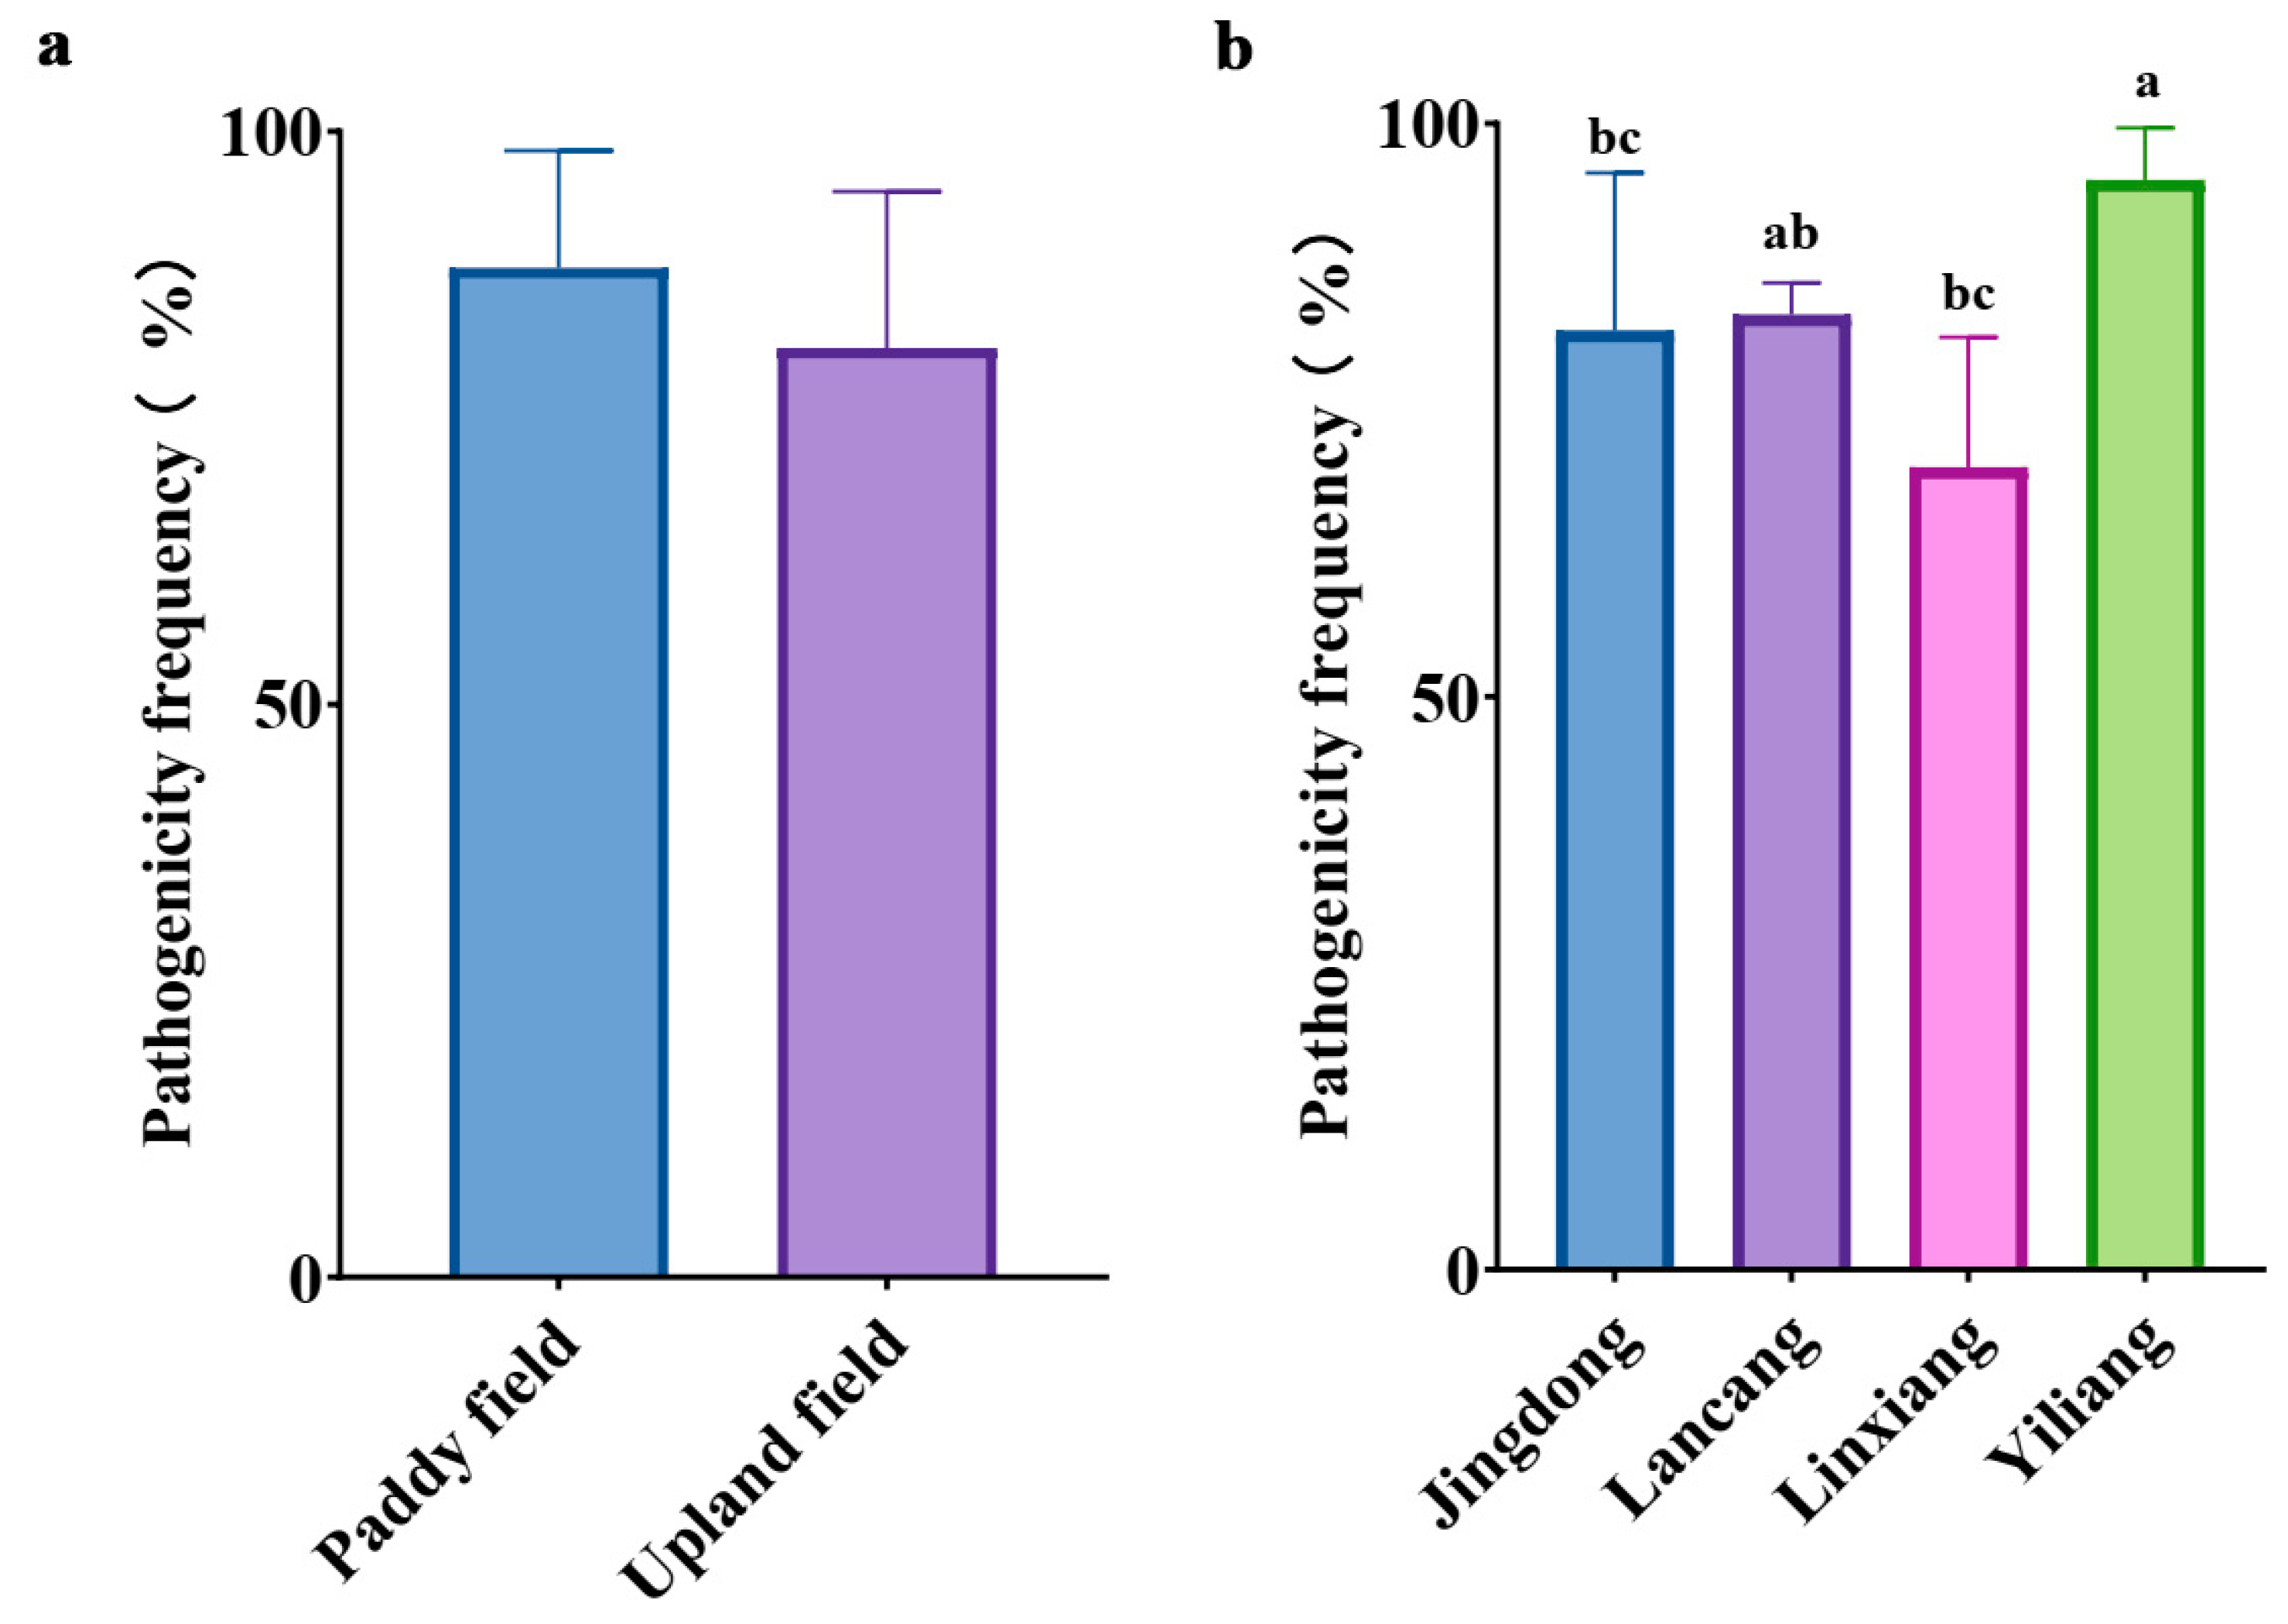
We compared the pathogenicity frequencies of the collected isolates from different planting fields and areas (Figure 1). However, there were no significant differences among the isolates from different planting fields, and the pathogenicity of isolates from Linxiang was significantly lower than that of isolates from Yiliang.
Figure 1.
Pathogenicity frequencies of collected isolates from different planting fields and areas. (a) The pathogenicity frequency of whole isolates from paddy and upland fields. (b) The pathogenicity frequency of whole isolates from four locations. Statistically significant differences were calculated by ANOVA Duncan’s test. Error bars represent the means ± SD. The different letters above each bar graph indicate significant differences (p < 0.05) among various treatments.
3.2. Resistance Assessment of Different Rice Varieties
We used the monogenetic lines and elite varieties to evaluate their resistant type in response to the 24 isolates. For the monogenetic lines, the disease resistance frequencies ranged from 8.33% to 70.83%, and the variety IRBL9-W with resistant gene Pi9 showed an incompatible reaction against 17 isolates (Table 3). The disease resistance frequencies of the other monogenetic varieties were less than 50%. Our results indicated that almost major R-gene-controlling varieties might be easily conquered by blast isolates from Dianheyou 615.
Table 3.
Resistance frequency of monogenetic lines in response to M. oryzae.
We also used 11 local varieties and commercial upland varieties for resistance identification. The disease-resistance frequencies ranged from 8.33% to 83.33%, and Diantun 506 showed the highest disease-resistance frequency (Table 4). The resistance frequencies of Lvhan 1, Linhan 1, Ridao 1, and Danzaodao were over 50%, while those of the other six varieties were less than 50%. These results suggested that some commercial varieties have better resistance to these blast isolates.
Table 4.
Resistance frequency of commercial rice varieties in response to M. oryzae.
3.3. Inhibitory Tests of Osmotic Stress and Fungicide in 24 Isolates
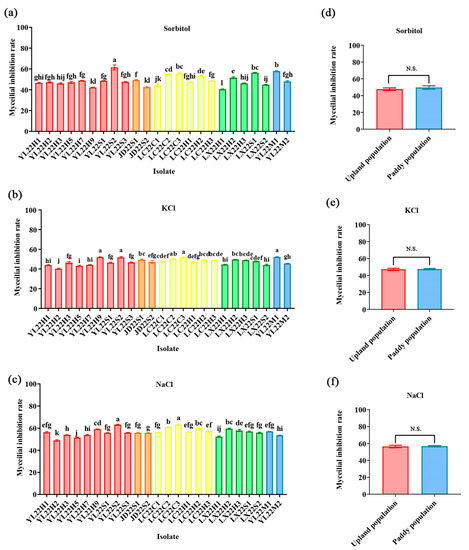
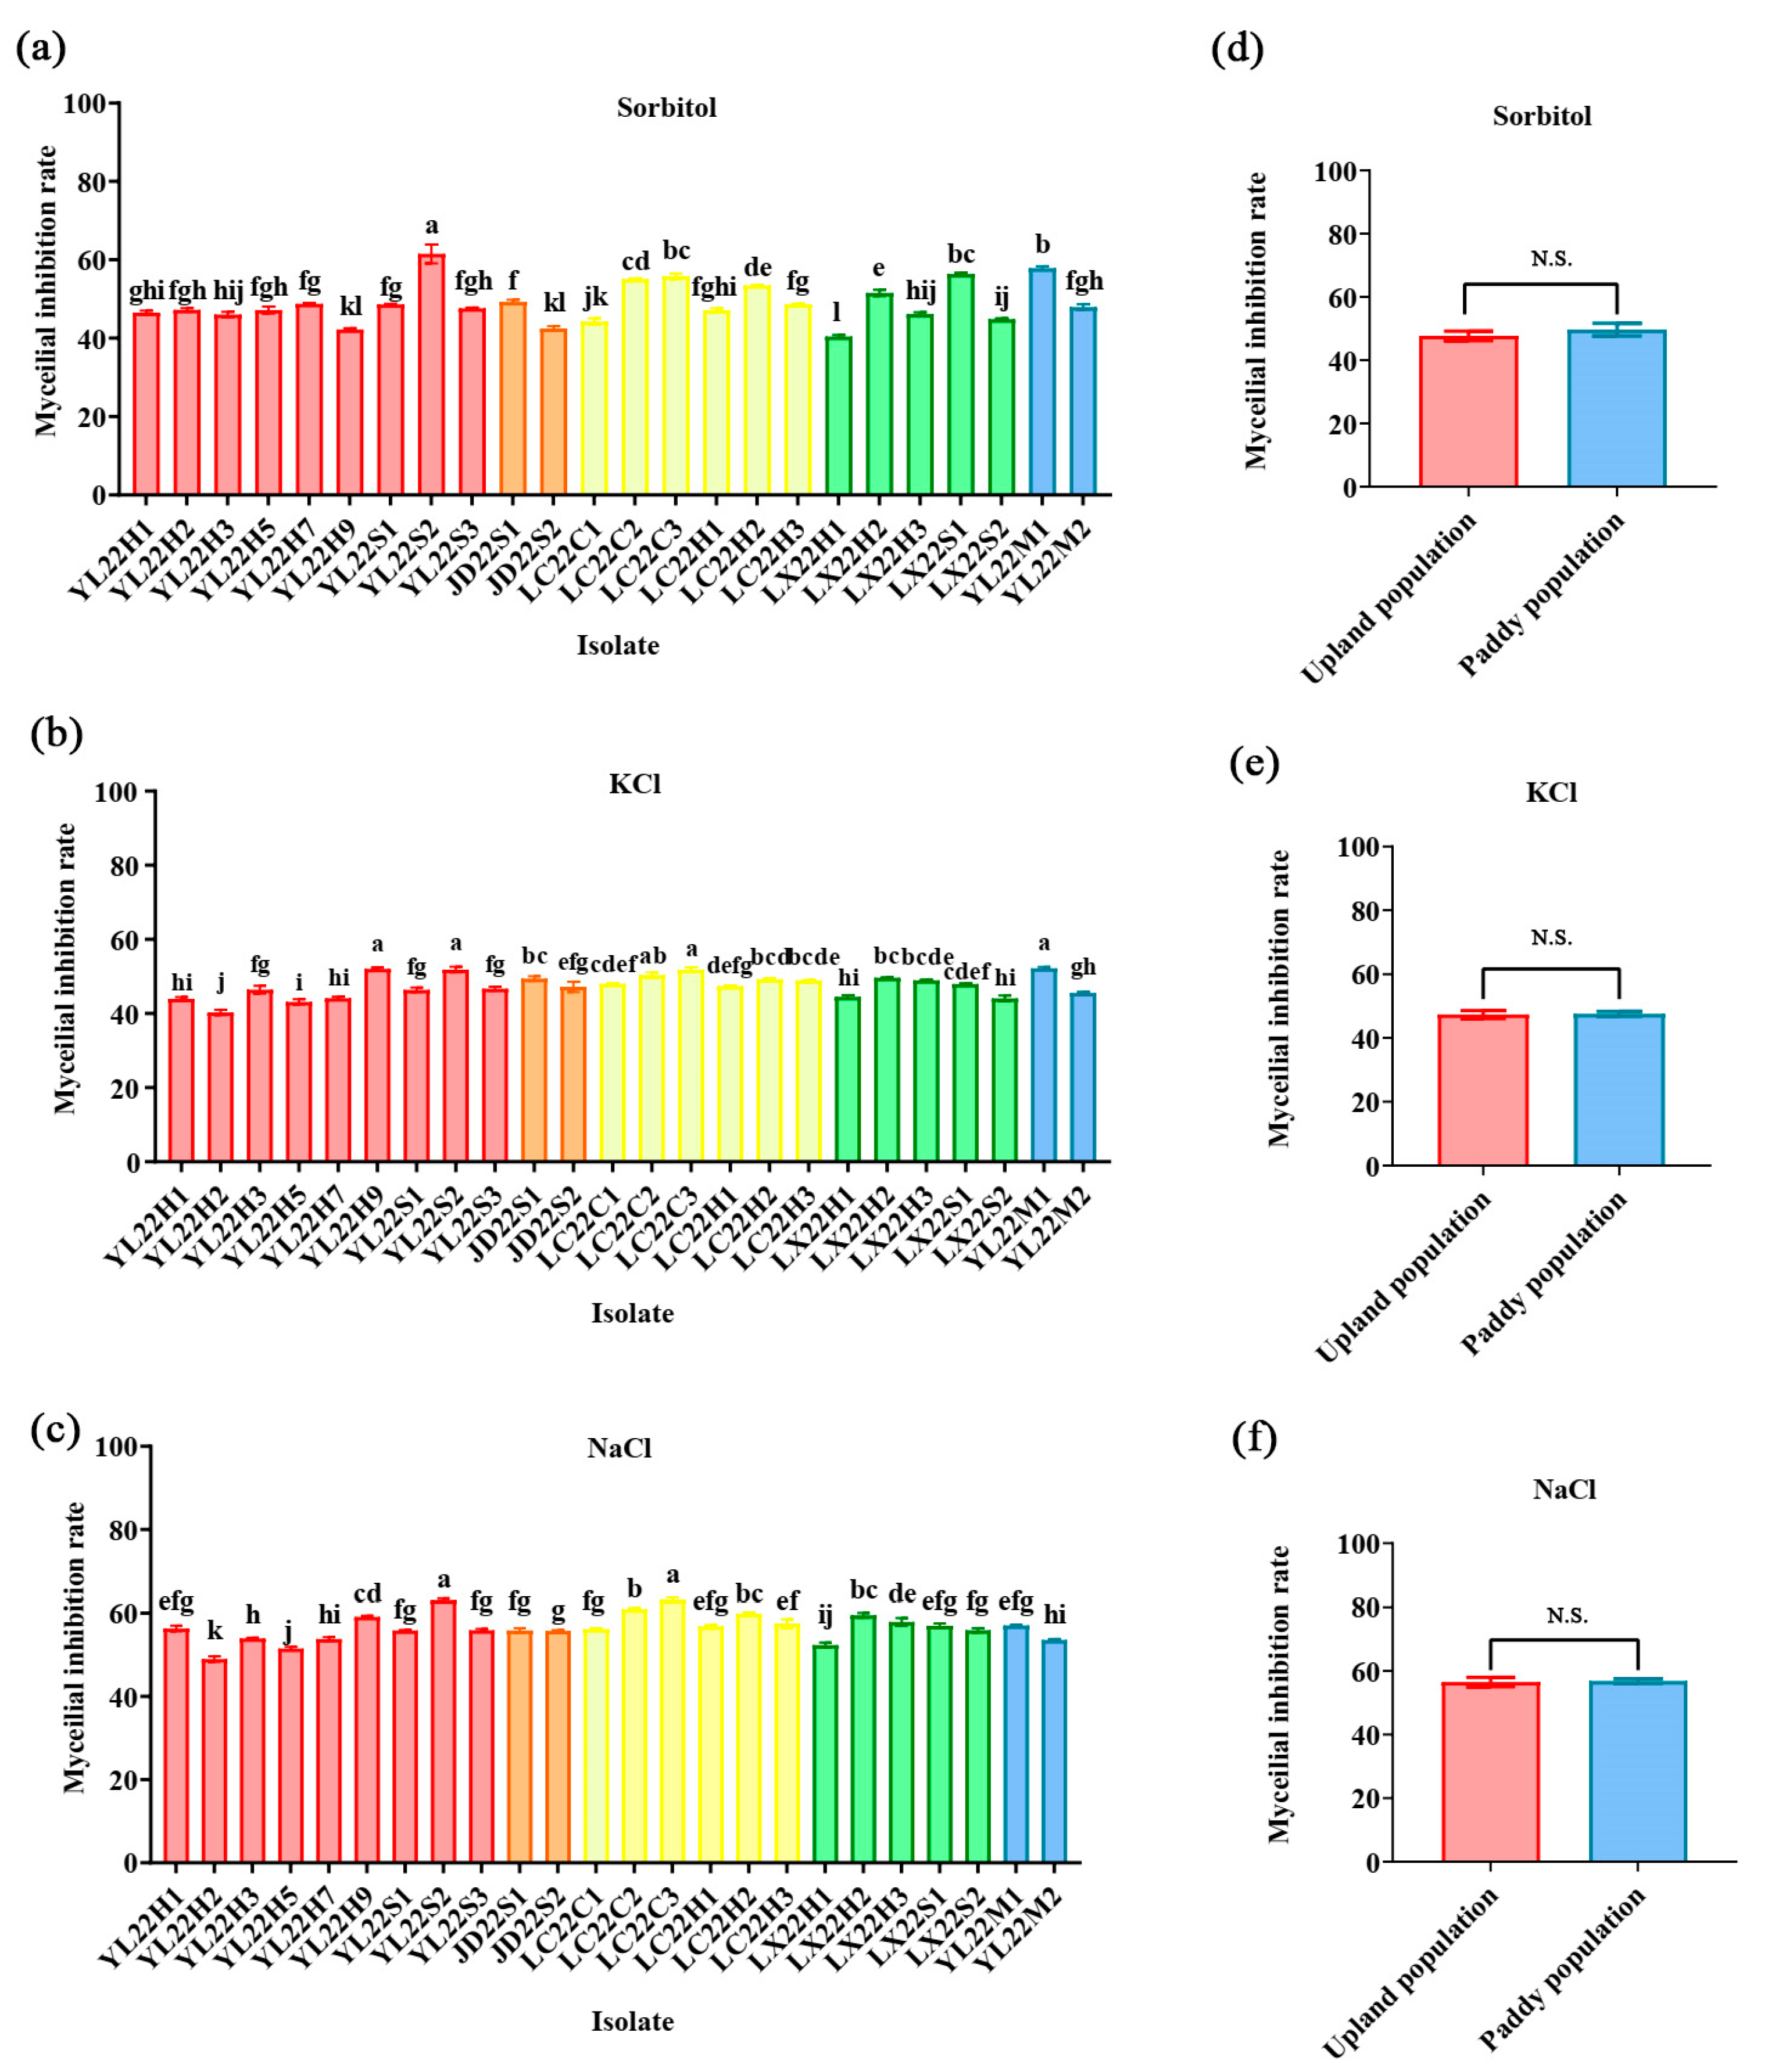
We tested the mycelial growth of the 24 isolates under excess sorbitol, KCl, and NaCl treatment. For the sorbitol treatment, the inhibitory rates were 40.45 ± 0.50% to 61.50 ± 2.40%, and the isolate YL22S2 from paddy rice was inhibited the most (Figure 2a). The inhibitory rates of KCl were 40.29 ± 0.72% to 52.19 ± 0.37%, and the isolate YL22M2 from D. sanguinalis was inhibited the most (Figure 2b). The inhibitory rates of NaCl were 49.00 ± 0.65% to 63.18 ± 0.54%, and the isolate LC22H3 from upland rice was inhibited the most (Figure 2c). However, there were no significant differences between the isolates from paddy and upland rice (Figure 2d–f).
Figure 2.
The inhibitory rates of collected isolates under sorbitol, KCl, and NaCl treatment. (a–c) The inhibitory rates of different isolates under treatment. (d–f) The inhibitory rates of paddy and upland populations under treatment. Statistically significant differences were calculated by ANOVA and Duncan’s test. Error bars represent the means ± SD. The different letters above each bar graph indicate significant differences (p < 0.05) among various treatments. N.S. means: no significant difference.
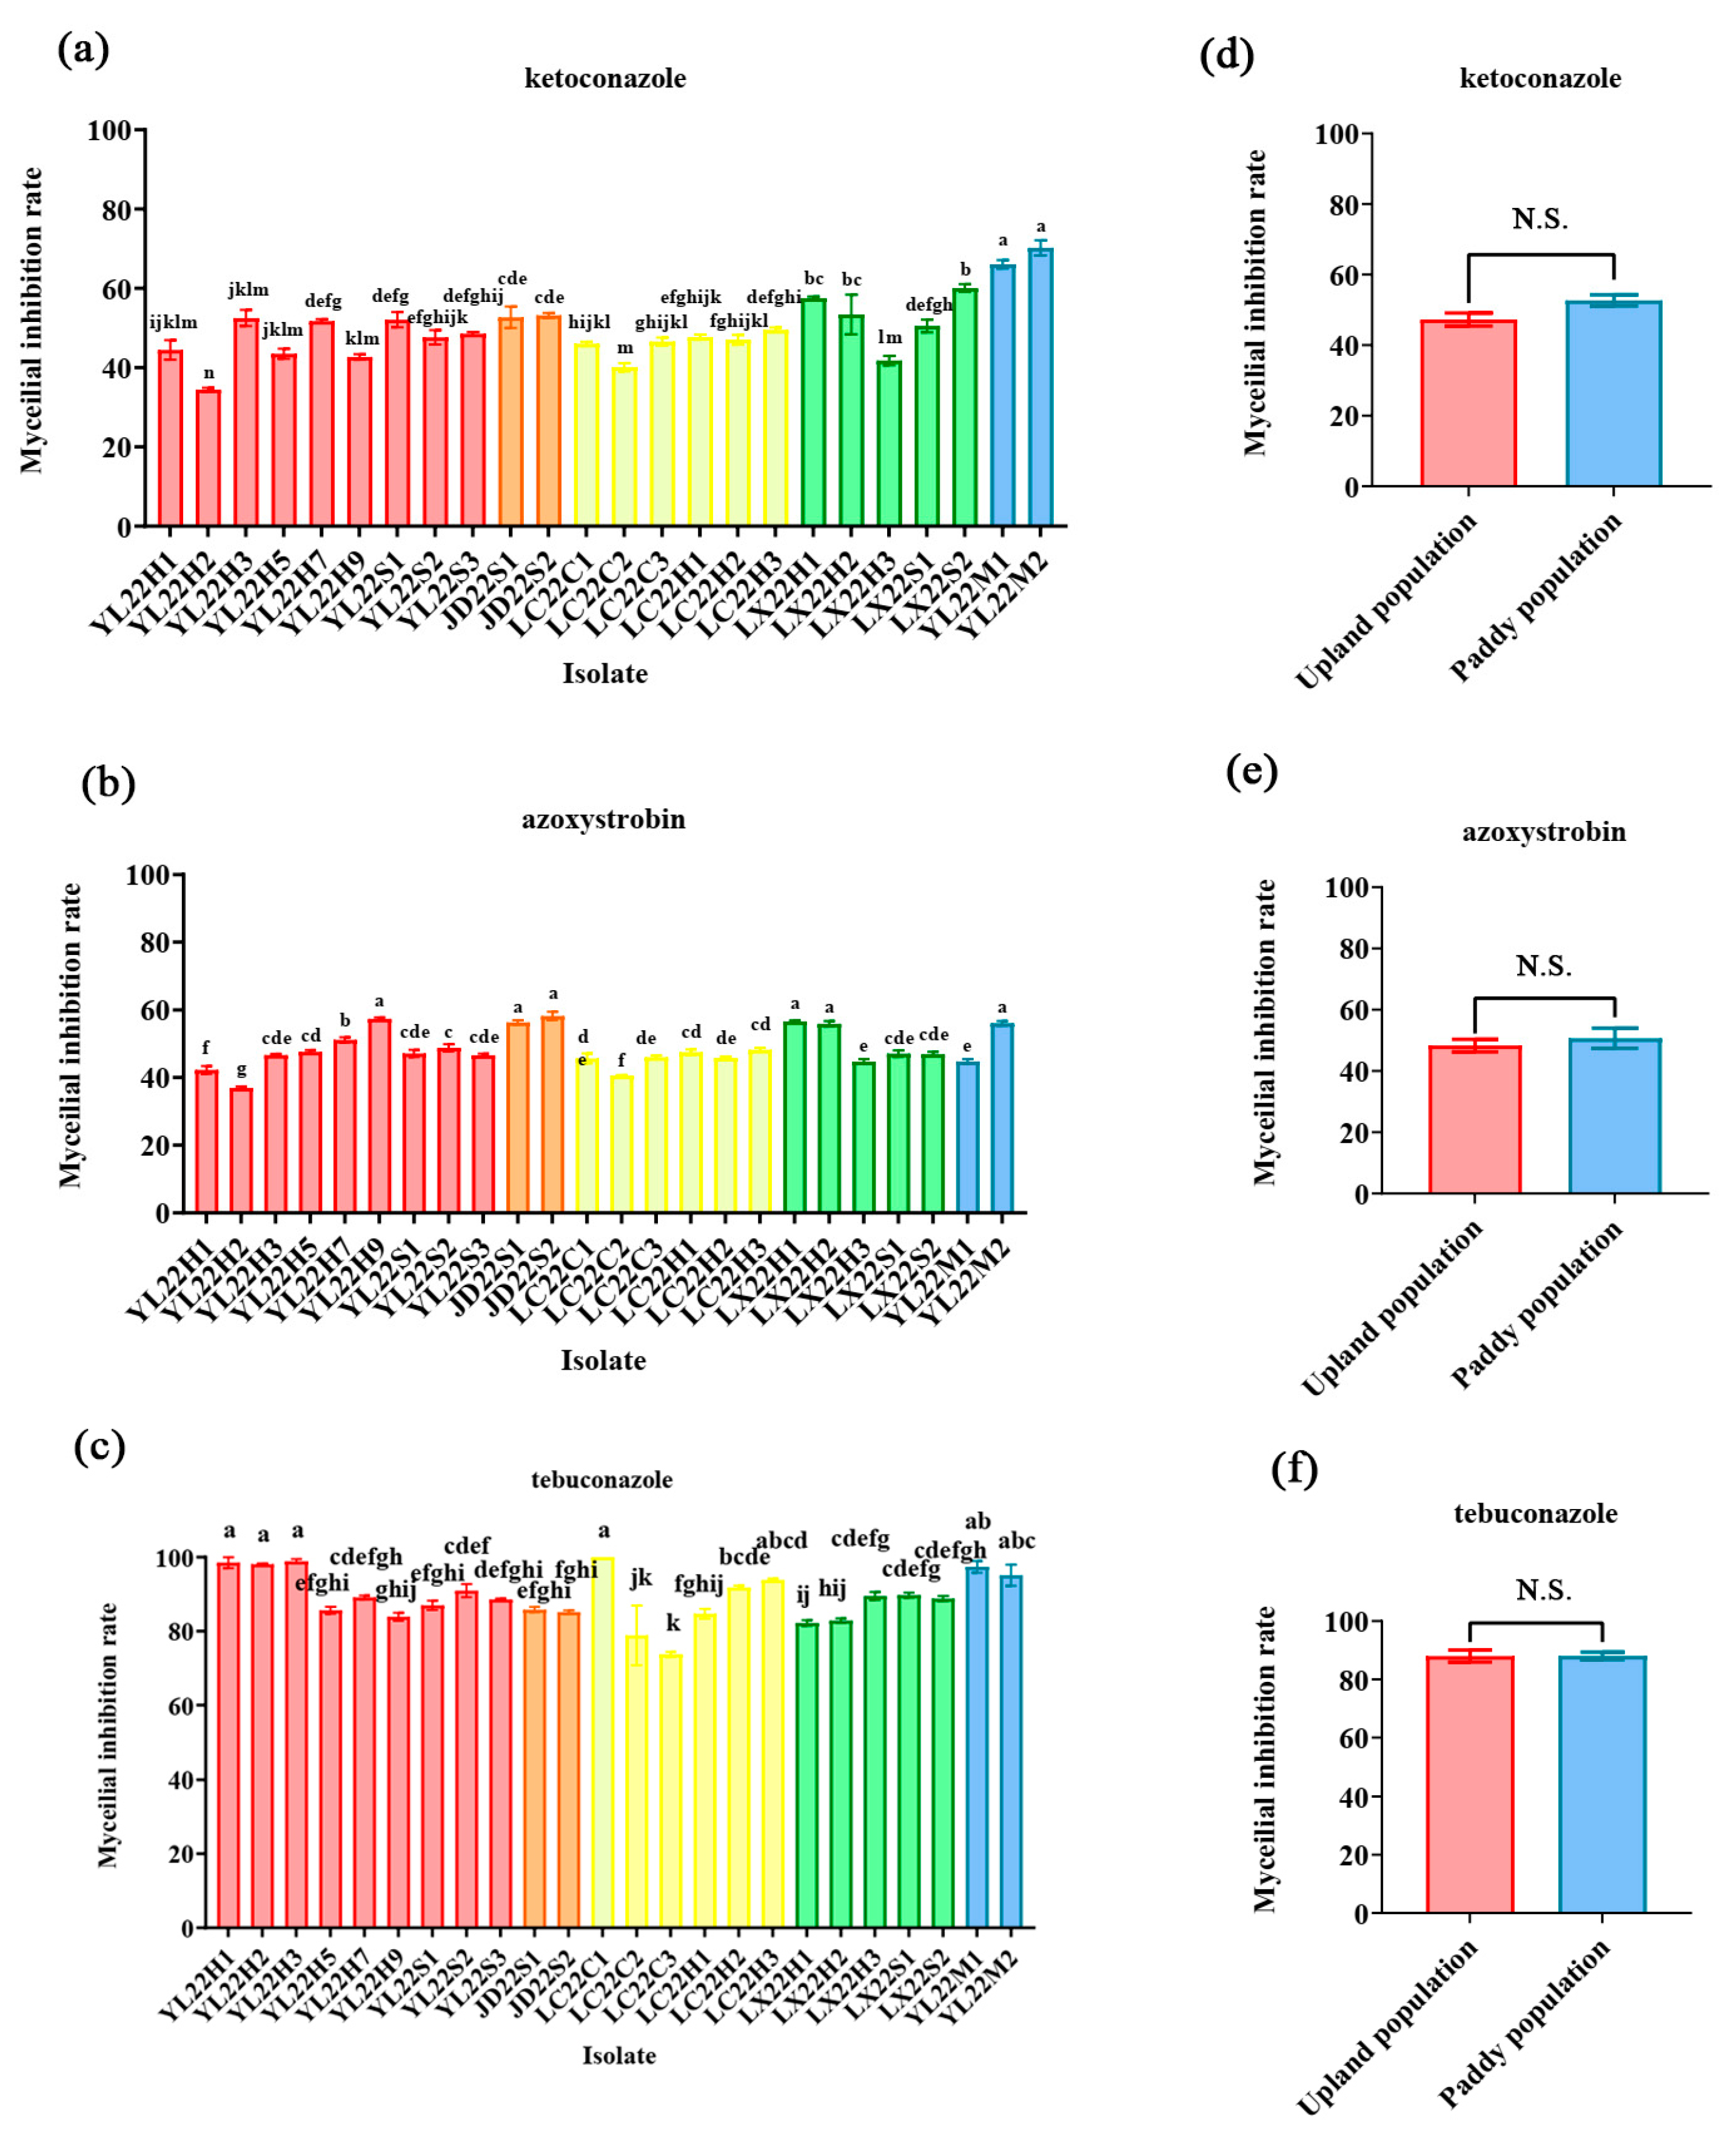
There were three fungicides, including ketoconazole, azoxystrobin, and tebuconazole, used for treatment, whose inhibitory rates were 34.49 ± 0.46% to 70.22 ± 1.92%, 36.96 ± 0.42% to 58.22 ± 1.21%, and 73.76 ± 0.68% to 100 ± 0.00% (Figure 3a–c). Similarly, the inhibitory rates of the three fungicides were not significantly different from the isolates from paddy and upland rice (Figure 3d–f).
Figure 3.
The inhibitory rates of collected isolates under fungicide treatment. (a–c) The inhibitory rates of different isolates under treatment. (d–f) The inhibitory rates of paddy and upland populations under treatment. Statistically significant differences were calculated by ANOVA and Duncan’s test. Error bars represent the means ± SD. The different letters above each bar graph indicate significant differences (p < 0.05) among various treatments. N.S. means: no significant difference.
3.4. Genome Sequencing and SNP Calling of 15 Representative Isolates
We selected 15 isolates from different hosts, planting fields, and locations for genome sequencing, including two Digitaria-infecting isolates (Table 5). For 13 rice-infecting isolates, the mean sequencing depth ranged from 29.16× to 49.56×, and the mapping rate ranged from 88.58% to 90.85%. There were 36,996 to 40,654 SNPs identified, the number of synonymous substitutions was 3306 to 3952, and that of non-synonymous substitutions was 4247 to 4518. For two Digitaria-infecting isolates, the mapping rates were 83.84% and 84.02%, and mean sequencing depths were 46.96× and 36.52×. Moreover, the SNPs of the two Digitaria-infecting isolates were much higher than those of rice-infecting isolates, which were 371,524 and 370,017.
Table 5.
The genomic variations in 15 sequenced isolates.
3.5. Polygenetic Analyses of 13 Sequenced Isolates
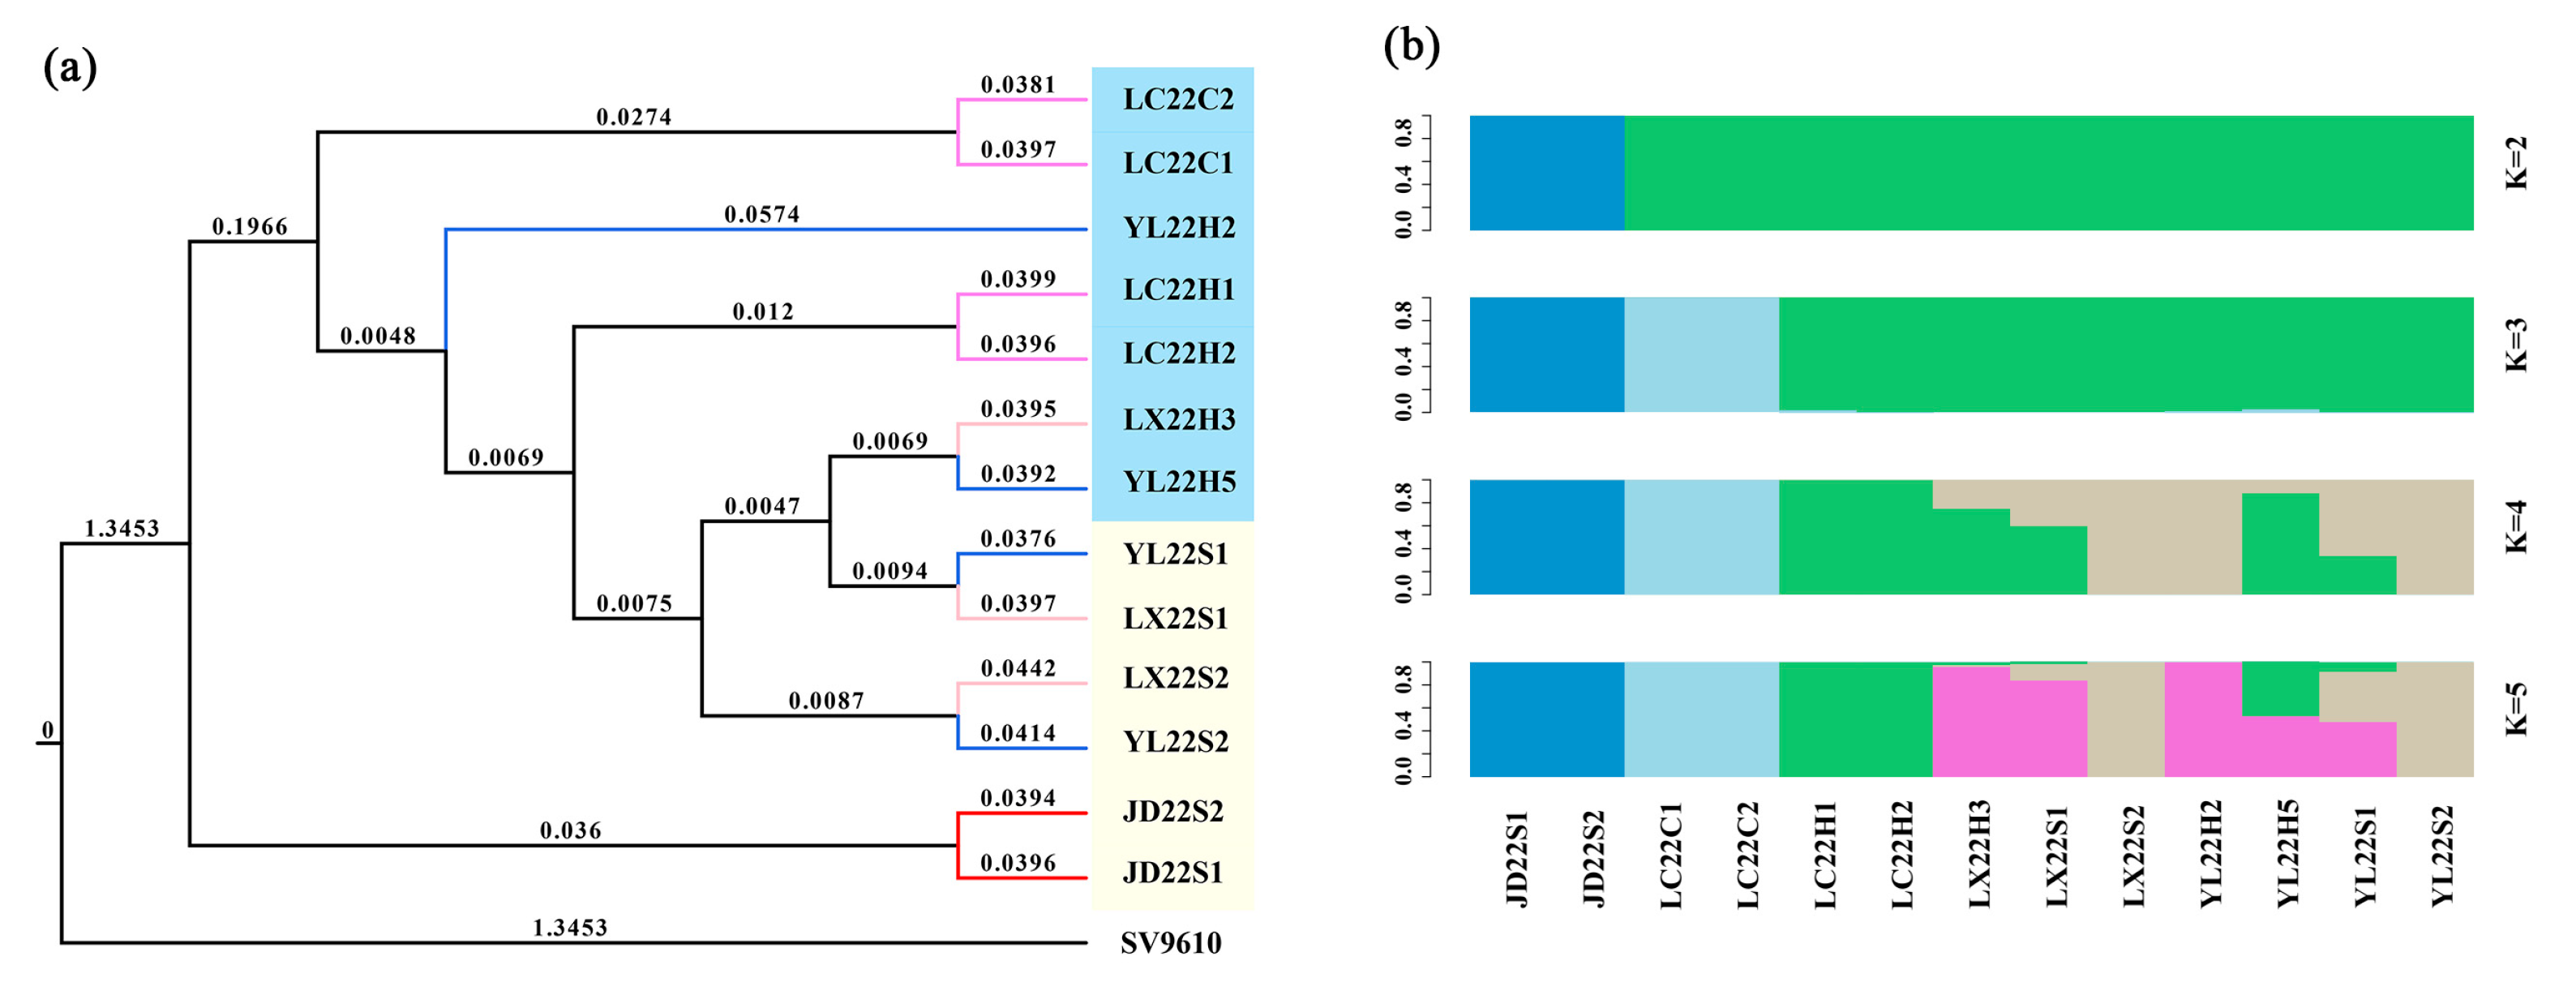
In order to characterize the genetic differences in the sequenced isolates from upland and paddy fields, we constructed a polygenetic tree based on the SNPs of 13 sequenced isolates and chose SV9610, a relative Setaria-infecting isolate, as the outgroup (Figure 4a). The two isolates collected from paddy fields in Jingdong were clustered together with geographic characteristics. Moreover, we found that some isolates from upland fields have closer relationships, most of which were from Lancang County, although one isolate was from Yiliang County. As for the other 6 isolates, they were collected in paddy and upland fields from Yiliang and Linxiang counties. We also evaluated the genetic structure of our samples according to the number of clusters (K) from 2 to 5 (Figure 4b). Jingdong-collected isolates from Dianheyou 615 in paddy fields were clustered together at K = 2, and the isolates from conventional upland varieties in Lincang were subdivided at K = 3. The isolates collected from Dianheyou 615 in upland fields from Lancang were separated at K = 5. Our results showed that there was no significant genetic difference between the isolates from paddy and upland fields, which might be caused by the short planting time of Dianheyou 615 in upland fields.
Figure 4.
The genetic differentiation of sequenced isolates from paddy and upland fields based on SNP analysis. (a). Ploygenetic tree of sequenced isolates. (b). Structure analysis of sequenced isolates. Different colors mean a closer genetic structure at various K values.
3.6. Functional Analyses of Planting-Filed Specific Genes Based on SNPs
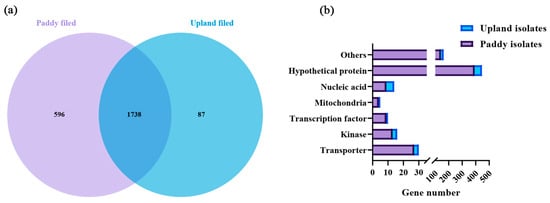
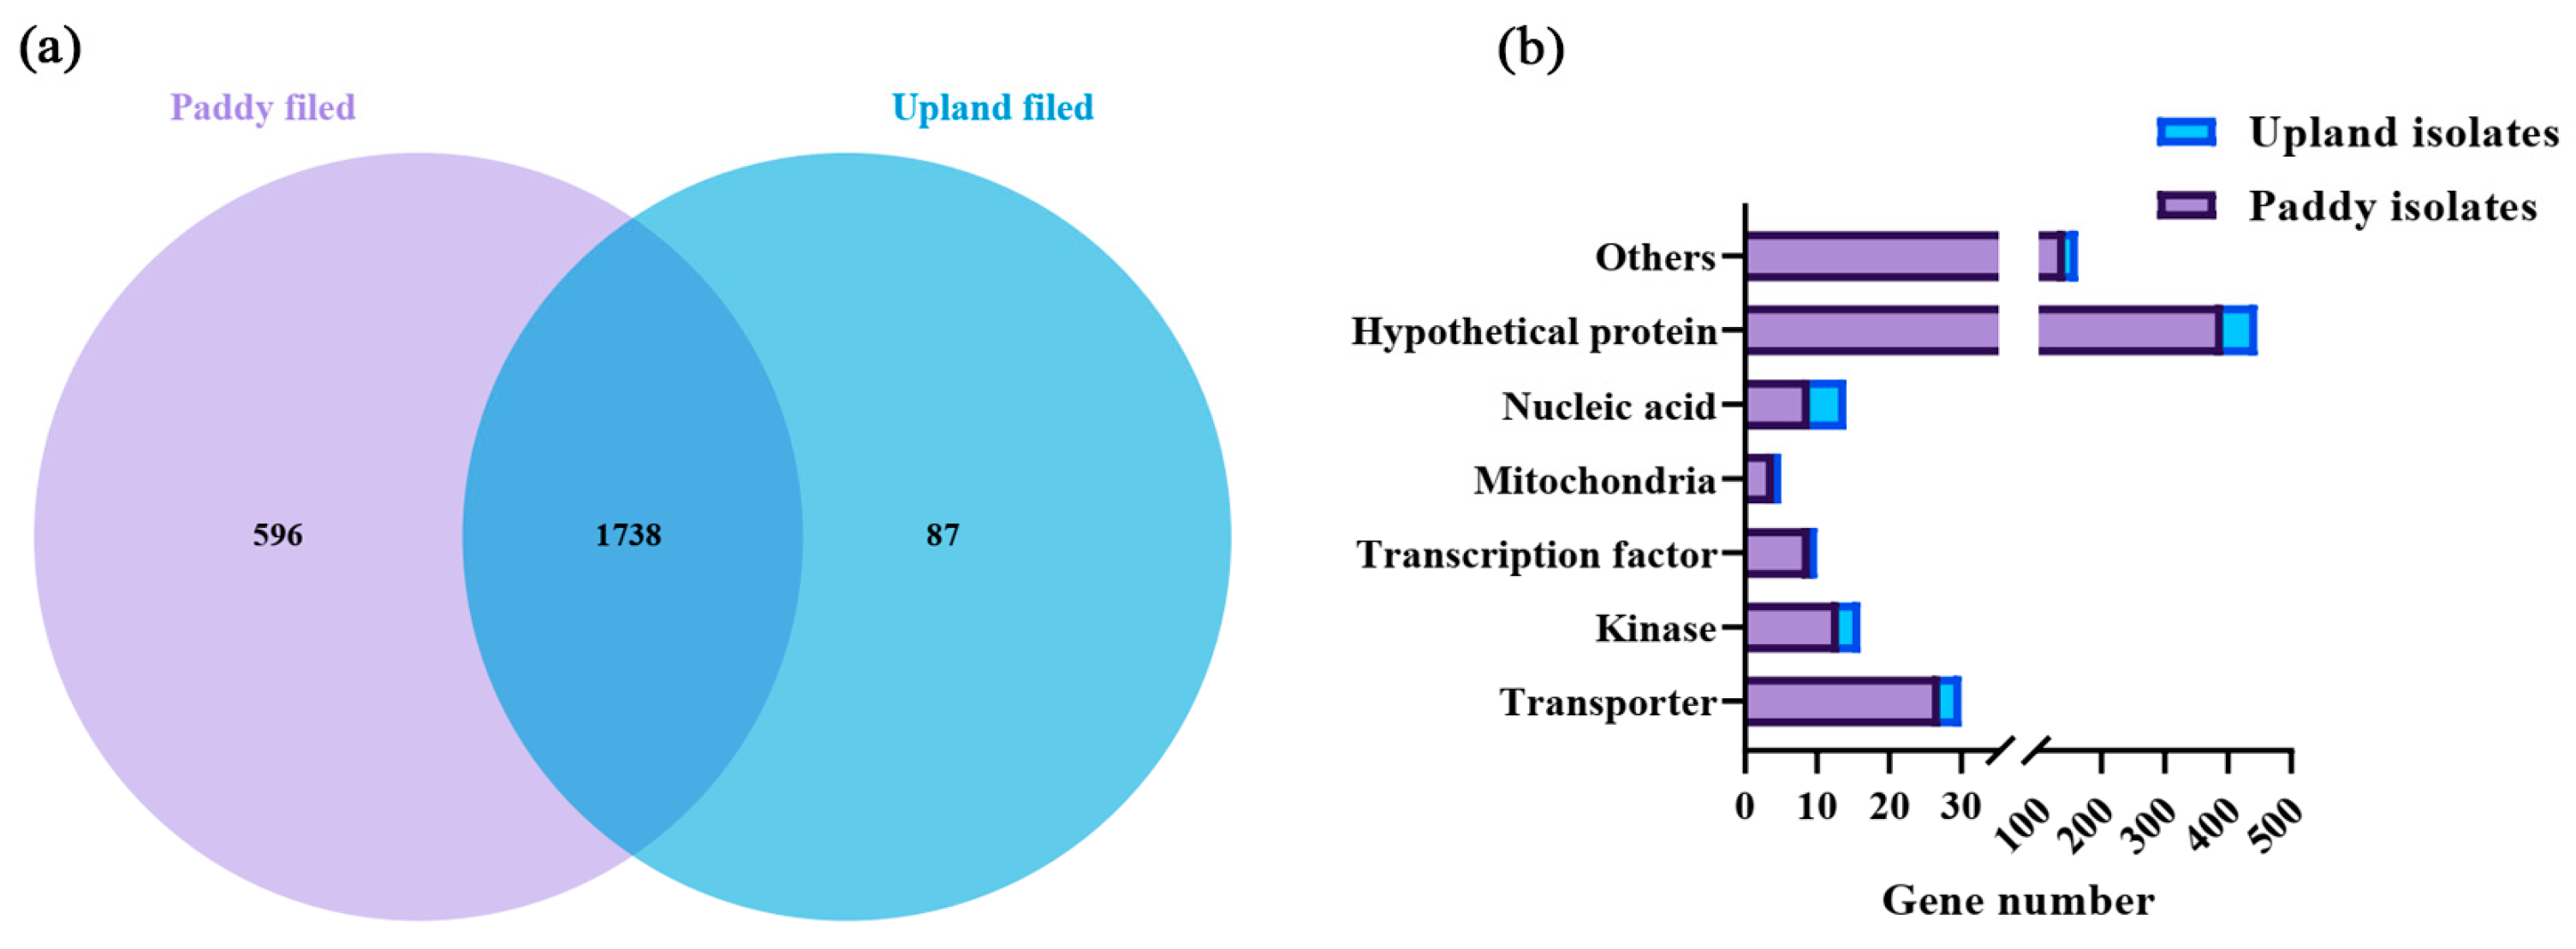
We integrated all exonic SNPs with non-synonymous substitution based on the genomes from paddy and upland isolates. There were 1738 genes with the same SNPs in both paddy and upland populations. A total of 596 and 87 genes were specifically found in paddy and upland populations (Figure 5a), respectively. We divided these genes into 7 functional groups, including transporter, kinase, transcription factor, mitochondria, nucleic acid, hypothetical protein, and others based on gene annotation. The number of paddy-specific genes was much greater than that of upland-population-specific genes in each functional group. Transporter- and kinase-related genes were the most found hypothetical protein among all the related groups (Figure 5b). Our results implied that the exchange of substance and signal transduction plays a major role in the division of paddy and upland populations.
Figure 5.
The SNP comparison of paddy and upland populations. (a) Venn plot showed the genes with exonic non-synonymous substitution SNPs among two populations. (b). The functional groups of SNP genes in paddy and upland populations.
4. Discussion
Water-saving and drought-resistant varieties are promising for rice breeding and cultivation [2]. Dianheyou 615, as an elite variety, can be planted in upland and paddy fields. High humidity in paddy fields aggravates disease occurrences, and many mechanisms were underlying. The Pseudomonas syringae effector HopM1 could improve the water content of apoplast under high humidity and favors the non-pathogenic P. syringae strain infection [11]. The transcription-activator-like effector (TALE) AvrHah1 in Xanthomonas gardneri activates a pectate lyase and promotes water uptake to enhance the tissue damage of tomato [12]. For rice blast disease, high ambient humidity promotes the development of infectious structures to enhance the virulence of blast fungus and reduces the activation of ethylene biosynthesis and signaling in rice [13,14,15]. In our results, we tested the pathogenicity of blast fungi from paddy and upland rice (Table 2). However, there were no significant differences in pathogenicity between the two groups (Figure 1a). In Yiliang County, the pathogenicity frequencies of paddy isolates were similar to those of upland isolates. However, the pathogenicity frequencies of paddy isolates seemed higher than those of upland isolates in Linxiang County, implying the possibility of pathogenicity changing according to the planting environment. The pathogenicity frequencies of upland isolates from Dianheyou 615 were also over 80%. Although high humidity influences disease occurrence, the pathogenicity frequencies of paddy and upland isolates were determined by comprehensive factors, including planting environment and local pathogen population.
In upland fields, the existence of weeds limits the growth of main crops. Many weeds can be infected by M. oryzae, and the different infecting lineages of M. oryzae have their own specific host plants [16]. Wheat-infecting lineage not only infects wheat but also infects other weed species [17]. Previous research showed that the long history of stable adaption between rice and rice-infecting lineage might decrease fungal genome diversity and gene number to develop host specificity [18]. However, recent results indicated that the Oryzae pathotype could infect wheat, implying the potential risk of host jump among various lineages [19]. We collected two Digitaria-infecting isolates from upland fields, and these two isolates could not infect monogenetic rice lines (Table 2), which is consistent with previous results [20]. Moreover, the genetic differentiation of Digitaria and rice-infecting isolates was significant. Our results indicated that the M. oryzae on Digitaria grass was not the source of infecting upland rice.
Many researchers have paid more attention to the population subdivisions of Oryzae pathotype isolates. Most results have indicated that there are three clonal lineages and one recombining lineage of rice blast fungus in the world, and Southeast Asia is the center of the origin, diversity, and dispersion of this fungus [8]. A recent result showed that partial specialization in rice subgroups and differences in the repertoires of putative virulence effectors caused the niche separation of these lineages and the loss of sex. Genetic incompatibilities limited the genetic flow between clonal lineages, maintaining the population subdivision [7]. In addition, the ecotypes of rice, such as indica and japonica rice, can change the blast occurrence in specific agrosystems [21]. The structure of multiple rice landraces also reshapes the pathogen population [22]. In our experiment, we wanted to explore the genetic variation between the isolates from one rice variety planted in paddy and upland fields. However, there were no significant differences between these two populations (Figure 4). We thought the area of paddy rice was much greater than that of upland rice in Yunnan and that most of the environment’s inoculums originated from paddy rice. The isolates of Dianheyou 615 in paddy and upland fields might be the offspring of paddy isolates. Although different planting environments could influence the physiology and metabolism of plants, which might develop specific defense responses, the short time of upland planting of Dianheyou 615 might not reshape the blast population and develop adapted interaction between upland rice and pathogens. Thus, genetic differentiation is not associated with the planting environment. Moreover, the lower number of sequenced isolates might also limit the analysis results. We also seem to have found some clues regarding SNP comparison between the two populations, and the upland-specific SNPs might accelerate the genetic subdivision of the upland population (Figure 5).
5. Conclusions
We found no significant differences in pathogenicity and stress response between the isolates from the rice variety Dianheyou 615 planted in paddy and upland fields. Genetic variations also indicated an indistinguishable relationship among these isolates from the two different planting environments examined in this study. Thus, the long-time collection of isolates from paddy and upland fields and the increased number of sequenced isolates would favor the exploitation of variation patterns of the two populations.
Author Contributions
Conceptualization, Y.W.; methodology, Z.W. and Y.S.; software, Q.W.; validation, C.W.; formal analysis, Y.G.; investigation, Z.W.; resources, L.G.; data curation, Q.W.; writing—original draft, Y.W.; visualization, X.P.; project administration, C.L. and Y.W.; funding acquisition, Y.W. All authors have read and agreed to the published version of the manuscript.
Funding
This research was supported by the National Natural Science Foundation of China (32202254, 32260711), Major Science and Technology Project of Yunnan and Kunming (202202AE090036), Basic Research Special Project in Yunnan (202101AU070101, 202201AT070255), Open Project of State Key Laboratory for Conservation and Utilization of Bio-Resources in Yunnan (gzkf2021010).
Data Availability Statement
The sequencing data were deposited at Sequence Read Archive with PRJNA948861.
Acknowledgments
We thank Fukuta and Dandan Li for providing rice materials.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Zhang, Q. Strategies for developing green super rice. Proc. Natl. Acad. Sci. USA 2007, 104, 16402–16409. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xia, H.; Zhang, X.; Liu, Y.; Bi, J.; Ma, X.; Zhang, A.; Liu, H.; Chen, L.; Zhou, S.; Gao, H. Blue revolution for food security under carbon neutrality: A case from the water-saving and drought-resistance rice. Mol. Plant 2022, 15, 1401–1404. [Google Scholar] [CrossRef] [Scilit]
- Luo, L. Breeding for water-saving and drought-resistance rice (wdr) in china. J. Exp. Bot. 2010, 61, 3509–3517. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xia, H.; Luo, Z.; Xiong, J.; Ma, X.; Lou, Q.; Wei, H.; Qiu, J.; Yang, H.; Liu, G.; Fan, L. Bi-directional selection in upland rice leads to its adaptive differentiation from lowland rice in drought resistance and productivity. Mol. Plant 2019, 12, 170–184. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dean, R.; Van Kan, J.A.; Pretorius, Z.A.; Hammond-Kosack, K.E.; Di Pietro, A.; Spanu, P.D.; Rudd, J.J.; Dickman, M.; Kahmann, R.; Ellis, J. The top 10 fungal pathogens in molecular plant pathology. Mol. Plant Pathol. 2012, 13, 414–430. [Google Scholar] [CrossRef] [Scilit]
- Gladieux, P.; Ravel, S.; Rieux, A.; Cros-Arteil, S.; Adreit, H.; Milazzo, J.; Thierry, M.; Fournier, E.; Terauchi, R.; Tharreau, D. Coexistence of multiple endemic and pandemic lineages of the rice blast pathogen. mBio 2018, 9, e01806–e01817. [Google Scholar] [CrossRef] [Scilit]
- Thierry, M.; Charriat, F.; Milazzo, J.; Adreit, H.; Ravel, S.; Cros-Arteil, S.; Borron, S.; Sella, V.; Kroj, T.; Ioos, R. Maintenance of divergent lineages of the rice blast fungus Pyricularia oryzae through niche separation, loss of sex and post-mating genetic incompatibilities. PLoS Pathog. 2022, 18, e1010687. [Google Scholar]
- Saleh, D.; Milazzo, J.; Adreit, H.; Fournier, E.; Tharreau, D. South-east asia is the center of origin, diversity and dispersion of the rice blast fungus, Magnaporthe oryzae. New Phytol. 2014, 201, 1440–1456. [Google Scholar] [CrossRef] [Scilit]
- Hayashi, N.; Fukuta, Y. Proposal for a new international system of differentiating races of blast (Pyricularia oryzae Cavara) by using LTH monogenic lines in rice (Oryza sativa L.). JIRCAS Work. Rep. 2009, 63, 11–15. [Google Scholar]
- Kadeawi, S.; Nasution, A.; Hairmansis, A.; Telebanco-Yanoria, M.J.; Obara, M.; Hayashi, N.; Fukuta, Y. Pathogenicity of isolates of the rice blast pathogen (Pyricularia oryzae) from Indonesia. Plant Dis. 2021, 105, 675–683. [Google Scholar] [CrossRef] [Scilit]
- Xin, X.-F.; Nomura, K.; Aung, K.; Velásquez, A.C.; Yao, J.; Boutrot, F.; Chang, J.H.; Zipfel, C.; He, S.Y. Bacteria establish an aqueous living space in plants crucial for virulence. Nature 2016, 539, 524–529. [Google Scholar] [CrossRef] [Scilit]
- Schwartz, A.R.; Morbitzer, R.; Lahaye, T.; Staskawicz, B.J. TALE-induced bHLH transcription factors that activate a pectate lyase contribute to water soaking in bacterial spot of tomato. Proc. Natl. Acad. Sci. USA 2017, 114, E897–E903. [Google Scholar] [CrossRef] [Scilit]
- Qiu, J.; Liu, Z.; Xie, J.; Lan, B.; Shen, Z.; Shi, H.; Lin, F.; Shen, X.; Kou, Y. Dual impact of ambient humidity on the virulence of Magnaporthe oryzae and basal resistance in rice. Plant Cell Environ. 2022, 45, 3399–3411. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Asibi, A.E.; Chai, Q.; Coulter, J.A. Rice blast: A disease with implications for global food security. Agronomy 2019, 9, 451. [Google Scholar] [CrossRef] [Scilit]
- Wilson, R.A.; Talbot, N.J. Under pressure: Investigating the biology of plant infection by Magnaporthe oryzae. Nat. Rev. Microbiol. 2009, 7, 185–195. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gladieux, P.; Condon, B.; Ravel, S.; Soanes, D.; Maciel, J.L.N.; Nhani Jr, A.; Chen, L.; Terauchi, R.; Lebrun, M.-H.; Tharreau, D. Gene flow between divergent cereal-and grass-specific lineages of the rice blast fungus Magnaporthe oryzae. mBio 2018, 9, e01219-17. [Google Scholar] [CrossRef] [Scilit]
- Islam, M.T.; Gupta, D.R.; Hossain, A.; Roy, K.K.; He, X.; Kabir, M.R.; Singh, P.K.; Khan, M.; Rahman, A.; Rahman, M. Wheat blast: A new threat to food security. Phytopathol. Res. 2020, 2, 28. [Google Scholar] [CrossRef] [Scilit]
- Wu, Q.; Wang, Y.; Liu, L.-N.; Shi, K.; Li, C.-Y. Comparative genomics and gene pool analysis reveal the decrease of genome diversity and gene number in rice blast fungi by stable adaption with rice. J. Fungi 2022, 8, 5. [Google Scholar] [CrossRef] [Scilit]
- Shizhen, W.; Jiaoyu, W.; Zhen, Z.; Zhongna, H.; Xueming, Z.; Rongyao, C.; Haiping, Q.; Yanli, W.; Fucheng, L.; Guochang, S. The risk of wheat blast in rice–wheat co-planting regions in china: Moo strains of Pyricularia oryzae cause typical symptom and host reaction on both wheat leaves and spikes. Phytopathology 2021, 111, 1393–1400. [Google Scholar] [CrossRef] [Scilit]
- Zhong, Z.; Norvienyeku, J.; Chen, M.; Bao, J.; Lin, L.; Chen, L.; Lin, Y.; Wu, X.; Cai, Z.; Zhang, Q. Directional selection from host plants is a major force driving host specificity in Magnaporthe species. Sci. Rep. 2016, 6, 25591. [Google Scholar] [CrossRef] [Scilit]
- Ali, S.; Gladieux, P.; Ravel, S.; Adreit, H.; Meusnier, I.; Milazzo, J.; Cros-Arteil, S.; Bonnot, F.; Jin, B.; Dumartinet, T. Evolution of the rice blast pathogen on spatially structured rice landraces maintains multiple generalist fungal lineages. Mol. Ecol. 2023, ahead of print. [Google Scholar] [CrossRef] [Scilit]
- Liao, J.; Huang, H.; Meusnier, I.; Adreit, H.; Ducasse, A.; Bonnot, F.; Pan, L.; He, X.; Kroj, T.; Fournier, E. Pathogen effectors and plant immunity determine specialization of the blast fungus to rice subspecies. Elife 2016, 5, e19377. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2023 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).