Article

Impacts of Neltuma chilensis Invasion on Native Species Richness, Abundance and Forest Structure in Hyphaene thebaica (Doum Palm) Forests of Sudan’s Drylands


by
Hashim Adam Abdelkarim
1,2,
Ali Omer
3,4,*,
Adrienn Horváth
2 and
Dafa Alla Mohamed Dafa Alla Ahmed
3
1
Faculty of Forest Sciences and Technology, University of Gezira, P.O. Box 20, Wad Madani 21111, Sudan
2
Faculty of Forestry, University of Sopron, Bajcsy-Zsilinszky u. 4, H-9400 Sopron, Hungary
3
Faculty of Forestry, University of Khartoum, P.O. Box 32, Khartoum North 13314, Sudan
4
Department of Botany and Biodiversity Research, University of Vienna, Renwen 14, 1030 Vienna, Austria
*
Author to whom correspondence should be addressed.
Forests 2026, 17(10), 1150; https://doi.org/10.3390/f17101150
Submission received: 10 August 2026 / Revised: 16 September 2026 / Accepted: 23 September 2026 / Published: 25 September 2026
(This article belongs to the Section Forest Biodiversity)

Abstract

Neltuma chilensis (Mesquite) is one of the world’s most aggressive invasive woody species, and its ecological impacts have drawn increasing scientific attention, particularly in arid and semi-arid ecosystems. In Sudan, it is rapidly reshaping Hyphaene thebaica (Doum palm) forests, yet its effects on native forest ecosystems remain poorly quantified. This study aimed to: (i) assess tree species composition and structure; (ii) evaluate the impact of N. chilensis invasion on species richness and native species abundance in H. thebaica forests. A stratified random sampling approach was employed across 59 plots within three forests reserves, namely Alhelgi, Geli and Um Bashim. N. chilensis showed overwhelming dominance in Alhelgi and Geli forests, with the highest densities of 1314 and 605 trees ha−1, and accounting for 83% and 86% of total tree density, and relative abundance of 63% and 71% of total tree stems, respectively. In contrast, N. chilensis was absent in Um Bashim forest. H. thebaica was the dominant native tree species, with the highest Importance Value Index (IVI) of 137. A total of nine species, belonging to seven genera and six families, were recorded across the studied forests. Within the invaded forests, Pearson’s correlation showed that increasing in N. chilensis abundance significantly reduced species richness (R = −0.34, p = 0.021). While Kendall’s tau confirmed a significant decline in native species abundance at the community level (τ = −0.22, p = 0.036), increasing abundance of N. chilensis was associated with a reduction in native woody species abundance. At the individual species level, this negative effect was not statistically significant for most species, except for Vachellia nilotica, which showed a significant decline (τ = −0.28, p = 0.022). In addition, the findings reveal N. chilensis as a formidable and accelerating threat to Doum palm forests’ integrity. The study recommends integrated management strategies, including the control of N. chilensis and restoration of native vegetation, to safeguard these dryland ecosystems.

1. Introduction

Over the past few decades, the presence of invasive species in native plant communities has emerged as a global ecological concern [1,2]. These biological invasions often lead to the displacement of native species, resulting in reduced vegetation cover and diminished availability of ecological resources [3,4]. Forest invasive species are defined as non-native flora, fauna, and microorganisms introduced into forest ecosystems beyond their natural range, where they spread rapidly and become dominant, posing serious threats to biodiversity, native habitats, and ecosystem functioning [4,5,6]. As one of the major drivers of habitat degradation and species extinction, invasive species significantly alter ecosystem processes by modifying soil stability, increasing erosion, and reshaping plant community structure [7,8]. Furthermore, they can disrupt nutrient cycling, reduce forest productivity, and reduce native species abundance [3,9,10].
The dominance of invasive species often results in substantial shifts in forest community composition [3], and decline in essential ecosystem services [11], primarily due to their strong competitive advantage over native vegetation [3,9]. Consequently, early detection and rapid response strategies are critical to limiting their spread, while long-term management approaches are essential for restoring ecosystem integrity and supporting native species recovery [12].
Among invasive species, N. chilensis is recognized as one of the most aggressive wood invaders, particularly in arid and semi-arid ecosystems worldwide [2]. It forms dense stands, exhibits strong drought tolerance, and effectively outcompetes native vegetation, thereby causing significant adverse effects on ecosystem structure and biodiversity [5].
In Sudan, N. chilensis (Mesquite) has received increasing attention from both scientific and public communities. The species was first introduced in 1917 by the government botanist E. Massey for multiple purposes, including drought mitigation, livestock fodder production, ecological restoration, and fuelwood supply [13]. Historically, it is widely planted to combat desertification, stabilize sand dunes, and protect settlements from wind erosion [14]. Consequently, it expanded across several regions, including Kassala, the Gash Delta, northern Sudan, the Red Sea Coast, and later into the Gezira irrigation scheme [15]. However, despite its initial benefits, N. chilensis has increasingly become a major ecological concern due to uncontrolled spread into natural and plantation forests, where it forms dense monospecific stands or coexists with native species, often leading to ecosystem degradation [13]. It is currently recognized as one of the most widespread invasive plant species, posing significant ecological challenges [15].
Despite the rapid expansion of N. chilensis across Sudan (Figure 1), its ecological impacts on native H. thebaica (Doum palm) forest ecosystems remain poorly understood. Limited information is available on its effects on vegetation structure, species richness, abundance, and ecological dominance. This knowledge gap constrains the development of effective management and conservation strategies for sustaining dryland forest ecosystems. Therefore, this study investigates the impact of N. chilensis invasion on native tree species richness and abundance in Doum palm forests, with particular emphasis on H. thebaica. Specifically, it aims to (i) assess tree species composition and structure, and (ii) evaluate the impact of N. chilensis invasion on species richness and native species abundance in H. thebaica forests. Furthermore, we hypothesize that the invasion of N. chilensis has significant negative effects on native species’ richness and native species abundance.

2. Methods

2.1. Study Area

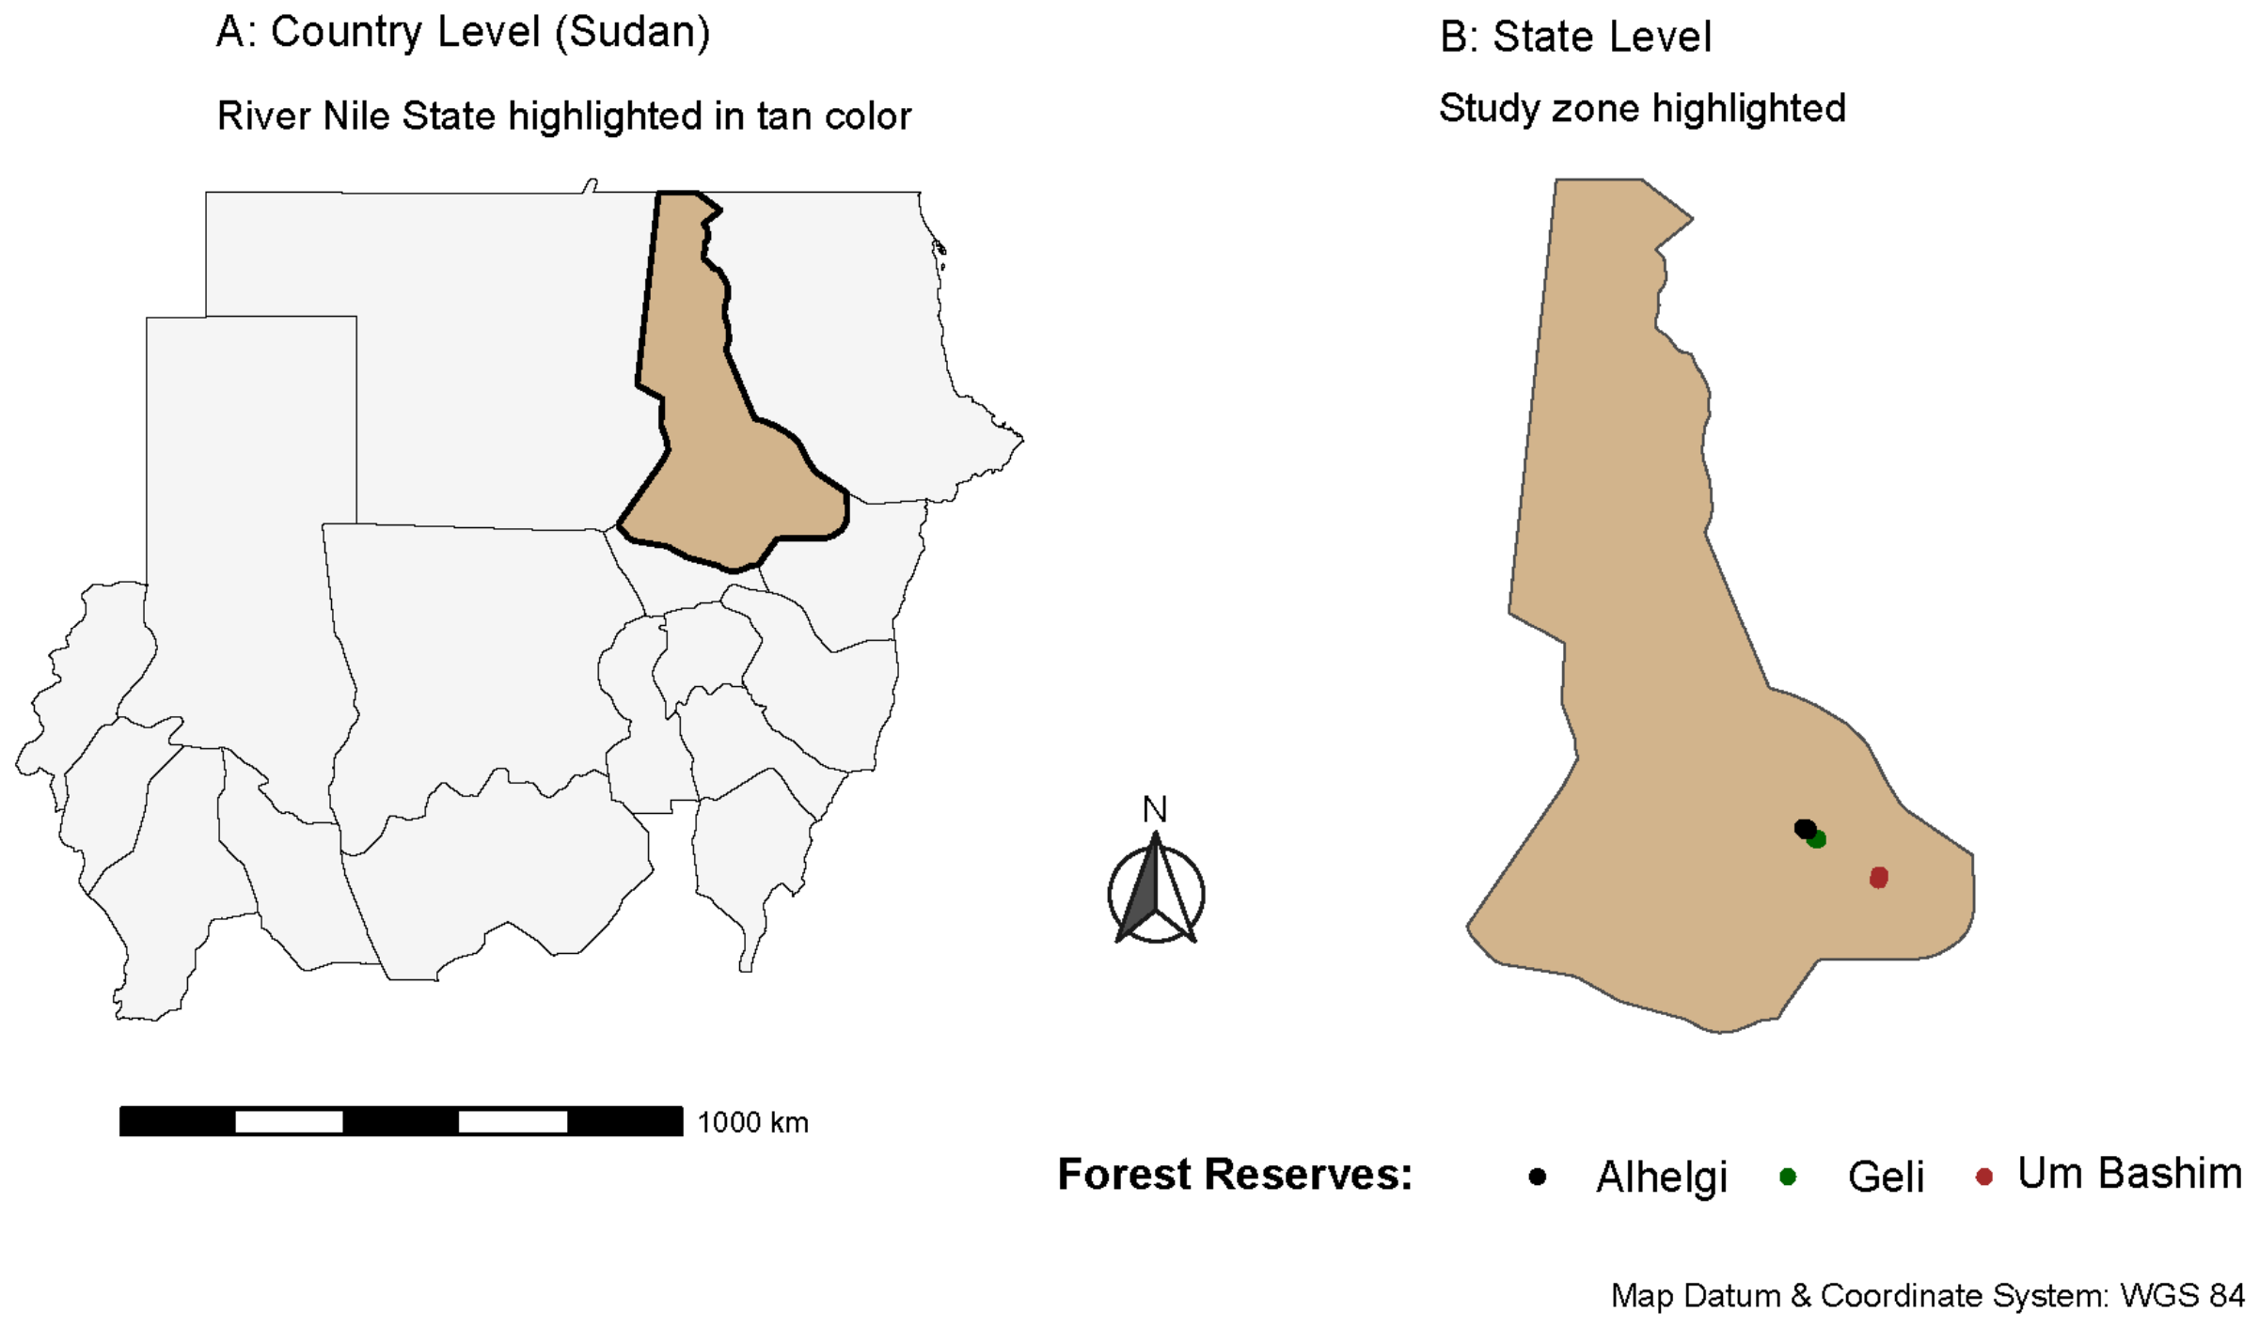
The study was conducted in El-Damar locality, River Nile State, Sudan (Figure 2), located between latitudes 16–22° N and longitudes 32–35° E [16]. The region covers approximately 124,000 km2 (12.4 million ha) and includes diverse dryland forest ecosystems distributed along riverbanks and seasonal watercourses. According to the Fifth Population Census, the state has a population of approximately 1,120,441, with an annual growth rate of 2.4% [17]. The climate is predominantly arid to semi-arid, characterized by extremely high temperatures and low, variable rainfall. Annual precipitation ranges from 0 to 25 mm in the northern parts to 100–150 mm in the southern areas, while mean maximum temperatures can reach up to 47 °C during summer, with minimum temperatures dropping to 8 °C in winter [16]. Vegetation is mainly restricted to riparian zones and areas influenced by seasonal water availability, where tree species such as Vachellia nilotica (Sunut), Vachellia oerfota (Laot), Vachellia seyal (Talih), Vachellia tortilis (Seyal), and Faidherbia albida (Haraz) are commonly found [17].

2.2. Sampling Design and Field Inventory

A stratified random sampling approach was employed across three Doum palm forest reserves: Um Bashim (208.3 ha), Geli (245.4 ha), and Alhelgi (674.8 ha). To account for spatial heterogeneity in vegetation structure, each forest reserve was stratified into four classes based on growing-stock density prior to field sampling. Remote sensing and Geographic Information System (GIS) techniques were used to characterize the spatial variation in growing-stock density. Satellite imagery was processed and analyzed using ArcGIS Pro 3.5, to identify and classify the spatial distribution of growing-stock density across the three forest reserves.
Based on the resulting density maps, each forest reserve was divided into four density classes representing a gradient from very low to high stand density. These classes were used as sampling strata, and sampling plots were randomly selected within each stratum to ensure adequate representation of vegetation and structural variation. Sampling plots were randomly allocated within each density stratum to adequately represent the spatial heterogeneity of vegetation across the forest reserves. Therefore, the number of plots differed among forest conditions, reflecting differences in the extent and variability of the density strata rather than a predefined equal allocation of plots between pristine and invaded forests. A total of 59 circular sampling plots (radius = 17.84 m; area ≈ 1000 m2 or 0.1 ha) were established, comprising 36 plots in Alhelgi, 12 plots in Geli, and 11 plots in Um Bashim. The total sampled area was therefore 5.9 ha. Given the combined forest area of 1128.5 ha, the overall sampling intensity was 0.52%.
Within each sampling plot, all woody plant individuals were identified to species level and counted, including seedlings, saplings, and mature plants. No minimum diameter at breast height (DBH) threshold was imposed, and DBH measurements were not recorded, as the study aimed to characterize species composition and abundance rather than forest structural attributes. The inclusion of all size classes was considered particularly important because several species, notably Neltuma chilensis, occurred predominantly as saplings with stem diameters of less than 5 cm. For each individual, species identity was recorded, and plot coordinates were obtained using a Global Positioning System (GPS) device. For each species, density and abundance were calculated using the total number of individuals recorded and the number of sampling plots in which the species occurred, respectively.

2.3. Floristic Composition and Species Identification

A comprehensive floristic survey was conducted to assess species composition at the family, genus, and species levels. Taxonomic classification followed the Angiosperm Phylogeny Group IV (APG IV) system [18]. Species identification was performed using standard references for Sudanese flora [19], supplemented by local ecological knowledge and relevant literature [18,20].
The nomenclature and taxonomic identities of all recorded plant species were verified and standardized using the current taxonomic databases Plants of the World Online (POWO) [21] and World Flora Online (WFO) [22]. Where alternative or previously used scientific names were encountered in the literature, the currently accepted names were adopted to ensure consistency throughout the manuscript. Accordingly, Prosopis chilensis was treated under its currently accepted name, Neltuma chilensis (Molina) C.E. Hughes & G.P. Lewis [23].

2.4. Data Analysis

Statistical analyses were conducted using SPSS (version 22), Microsoft Excel (version 16), and R software (version 4.5.1). Ecological parameters were calculated to quantify species composition and vegetation structure and distribution, including frequency (F), relative frequency (RF), density (D), relative density (RD), abundance (A), relative abundance (RA), and the Importance Value Index (IVI) (Table 1). These indices were computed following standard ecological methods [20,24,25,26].
Pearson’s correlation coefficient was used to evaluate the relationship between N. chilensis abundance and species richness. In addition, Kendall’s tau (τ), a non-parametric correlation measure suitable for small sample sizes and count data, was used to assess the association between N. chilensis abundance and native species abundance at both community and individual species levels.

3. Results

3.1. Species Composition, Vegetation Structure and Family Abundance in the Study Area

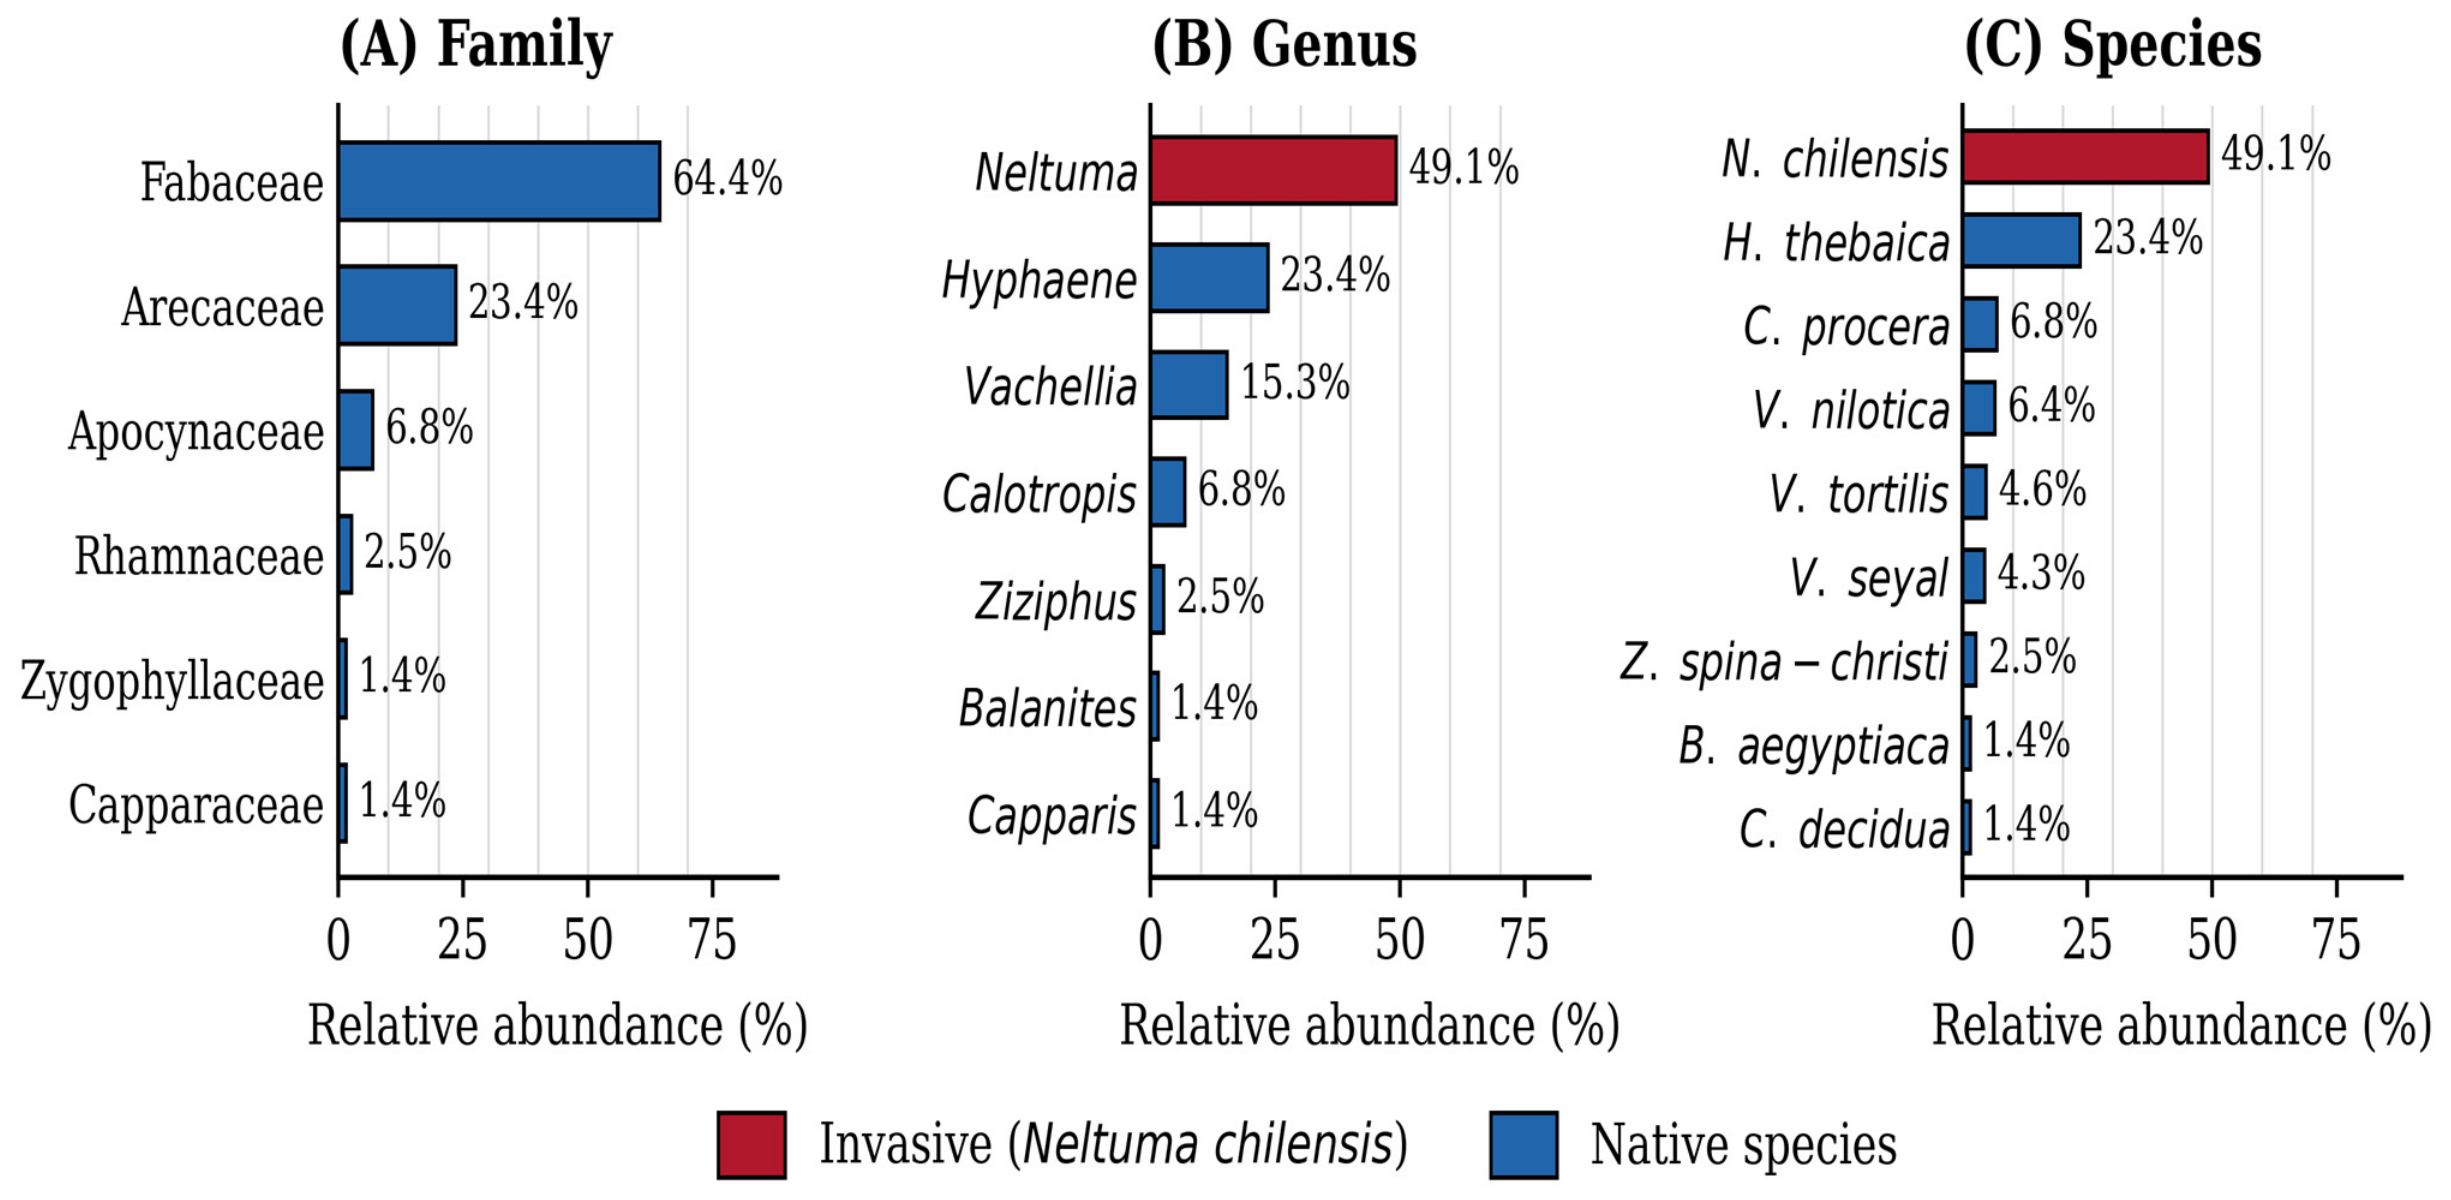
Vegetation structure and species composition differed markedly among the three forest reserves (Table 2). In Um Bashim Forest, H. thebaica (Doum palm) was the dominant species, exhibiting a density of 454 trees ha−1, a relative density of 66%, and the highest Importance Value Index (IVI = 137). The absence of N. chilensis and the dominance of H. thebaica indicate a structurally stable native forest in which the indigenous species maintains ecological dominance. In contrast, N. chilensis was the dominant species in both Alhelgi and Geli forests, exhibiting densities of 1314 and 605 trees ha−1, respectively, and accounting for 58%–66% of the total Importance Value Index (IVI; 175 and 197 out of a maximum of 300, respectively). Its exceptionally high density and IVI reflect strong ecological dominance, substantial displacement of native woody species, and pronounced alterations in forest composition and vegetation structure. A total of nine species belonging to seven genera and six families were recorded across the three forest reserves. Fabaceae was overwhelmingly the dominant family, accounting for 64.4% of total tree abundance, driven primarily by N. chilensis (Figure 3). This pattern indicates that the invasion of N. chilensis has substantially modified community composition by increasing the dominance of Fabaceae and reducing the relative importance of native woody species. While Figure 3 summarizes the overall taxonomic composition across the study area, site-specific composition and importance values are presented in Table 2.

3.2. Impact of N. chilensis on Native Species Richness and Abundance

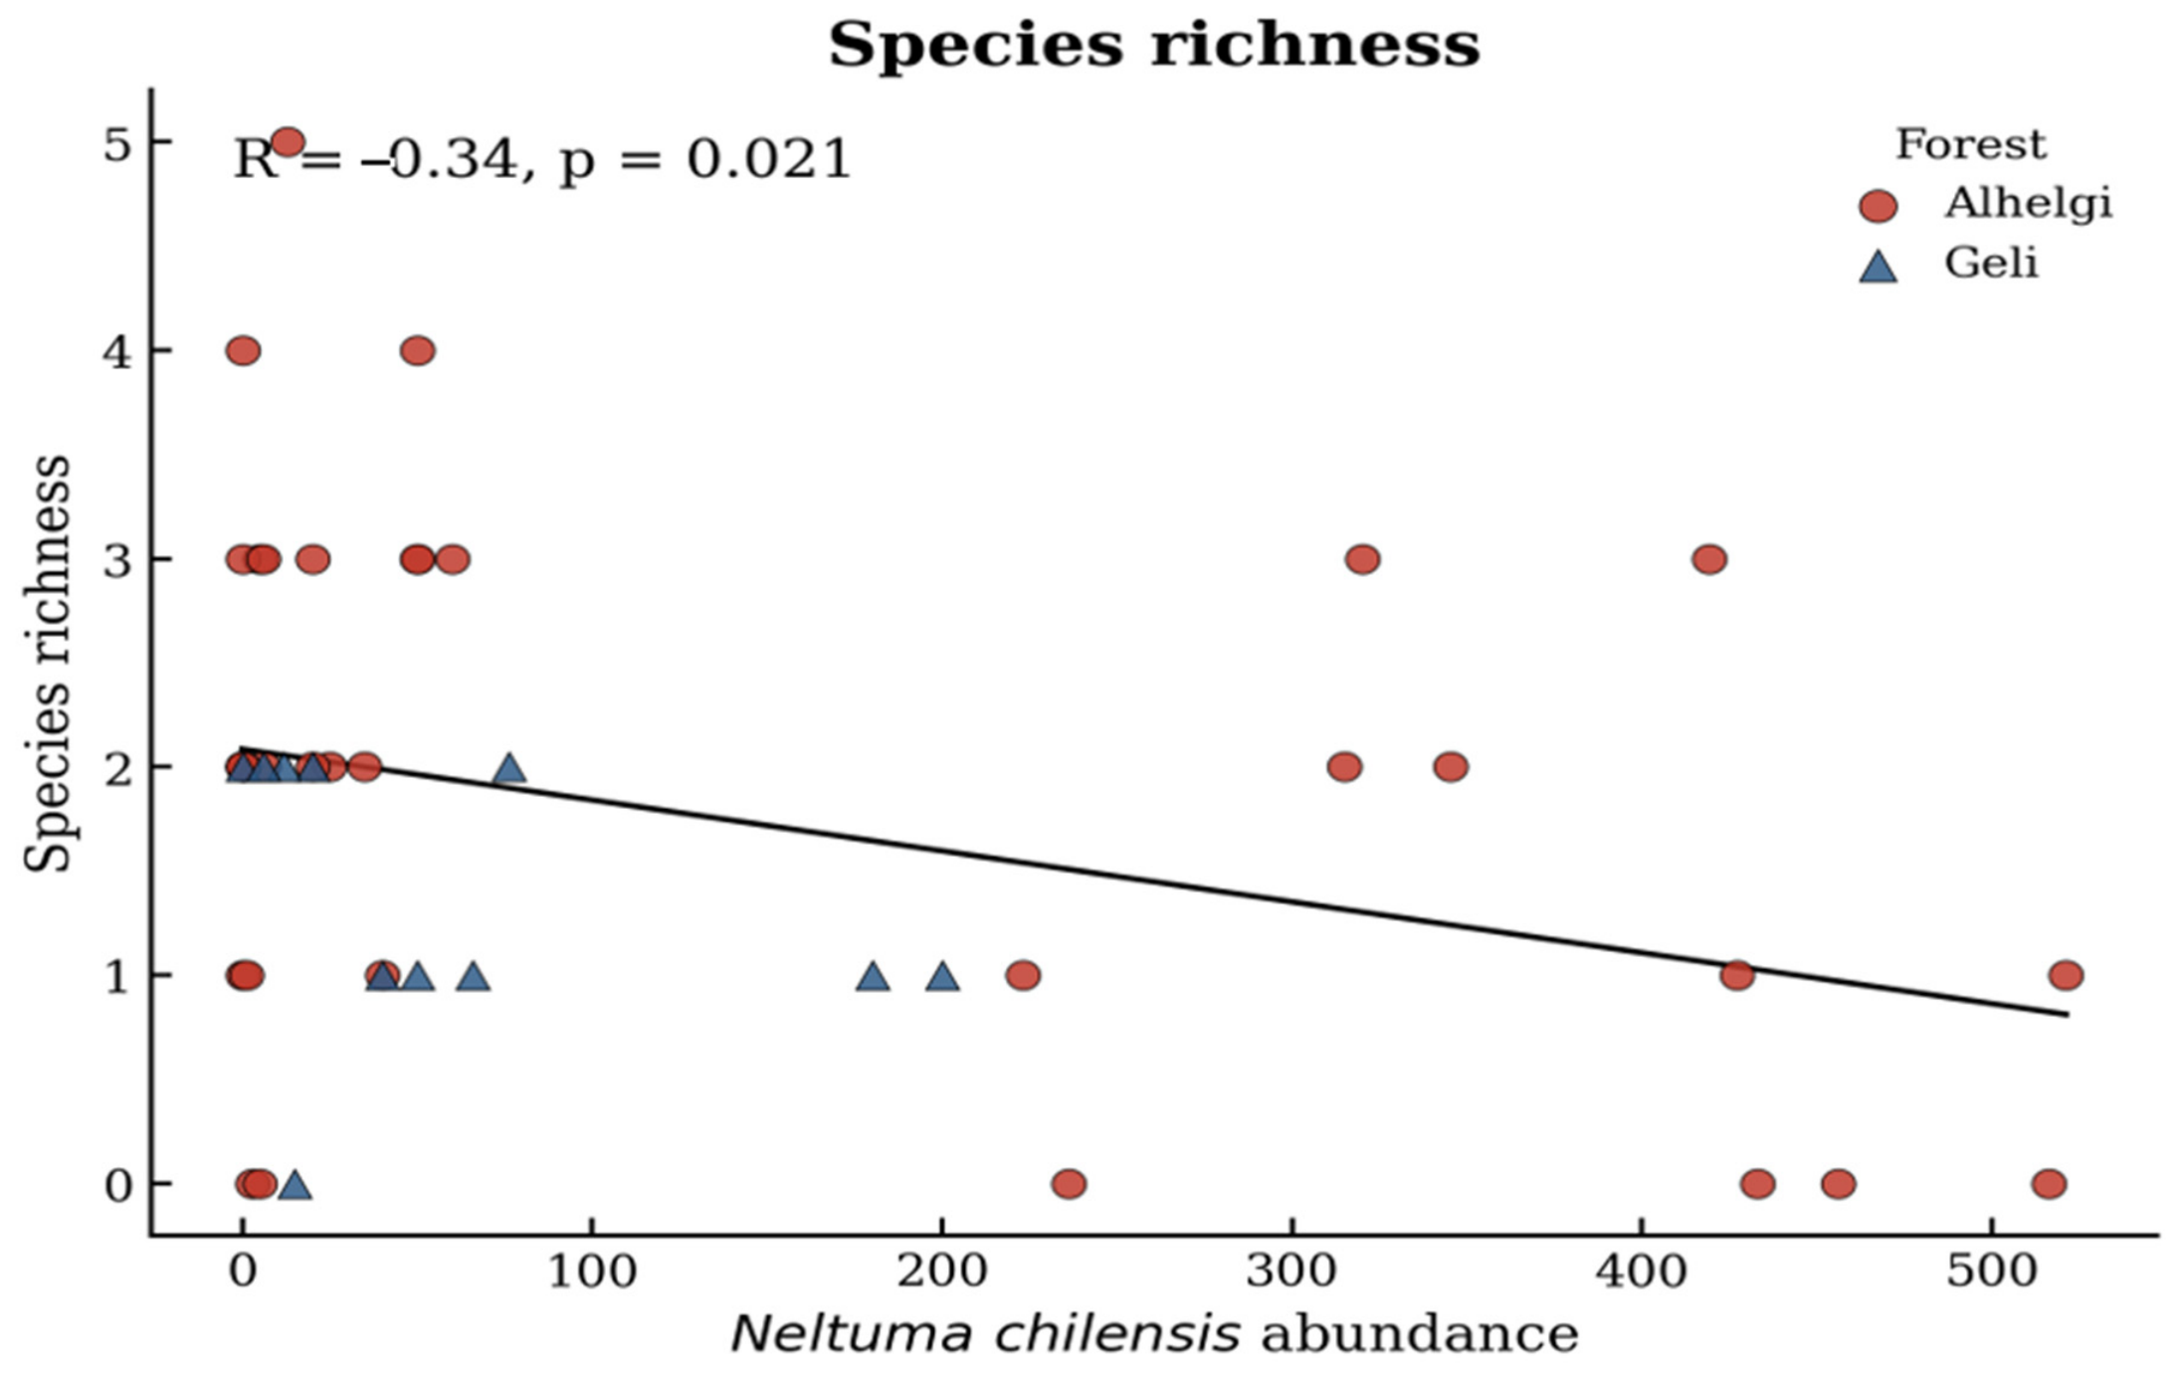
Species composition differed markedly among forest sites, reflecting varying levels of invasion and ecological conditions. A Pearson correlation analysis (Figure 4) revealed a significant negative relationship between N. chilensis abundance and native species richness (R = −0.34, p = 0.021); an increase in N. chilensis abundance was associated with a decline in species richness. N. chilensis is predominantly concentrated in Alhelgi and Geli forests, while it is completely absent in Um Bashim Forest, which is largely dominated by H. thebaica (Doum palm).
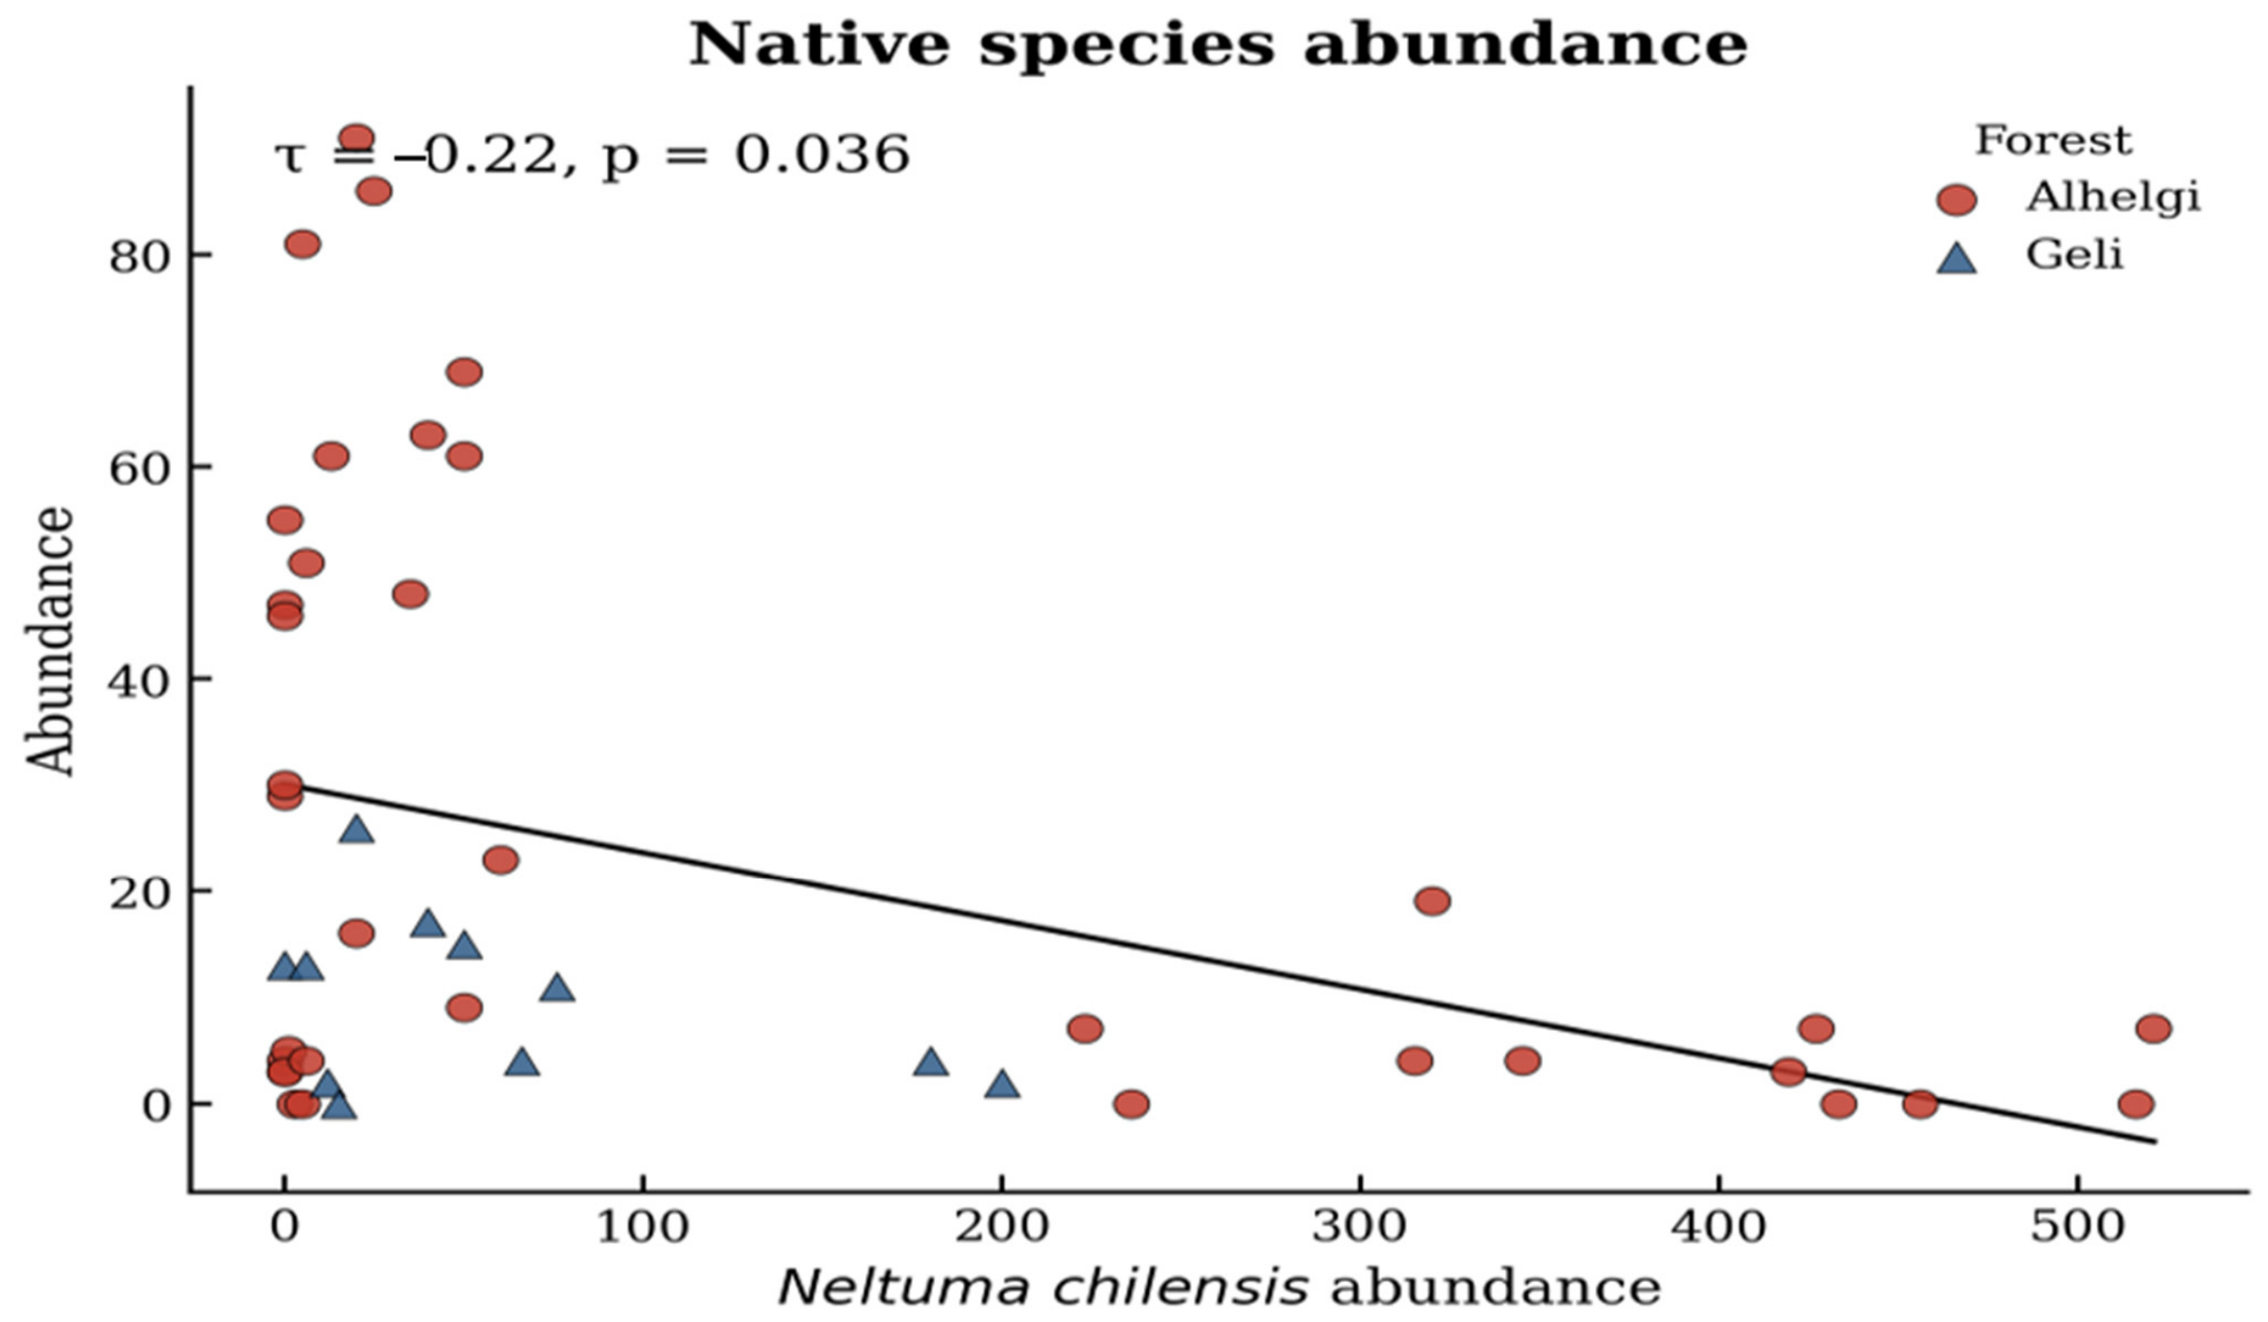
Kendall’s tau (τ) correlation analysis revealed a weak but statistically significant negative association between N. chilensis abundance and native species abundance at the community level (τ = −0.22, p = 0.036). This finding indicates that increasing abundance of N. chilensis is associated with a decline in native species abundance (Figure 5). The observed negative trend indicates an association between N. chilensis abundance and native species abundance.
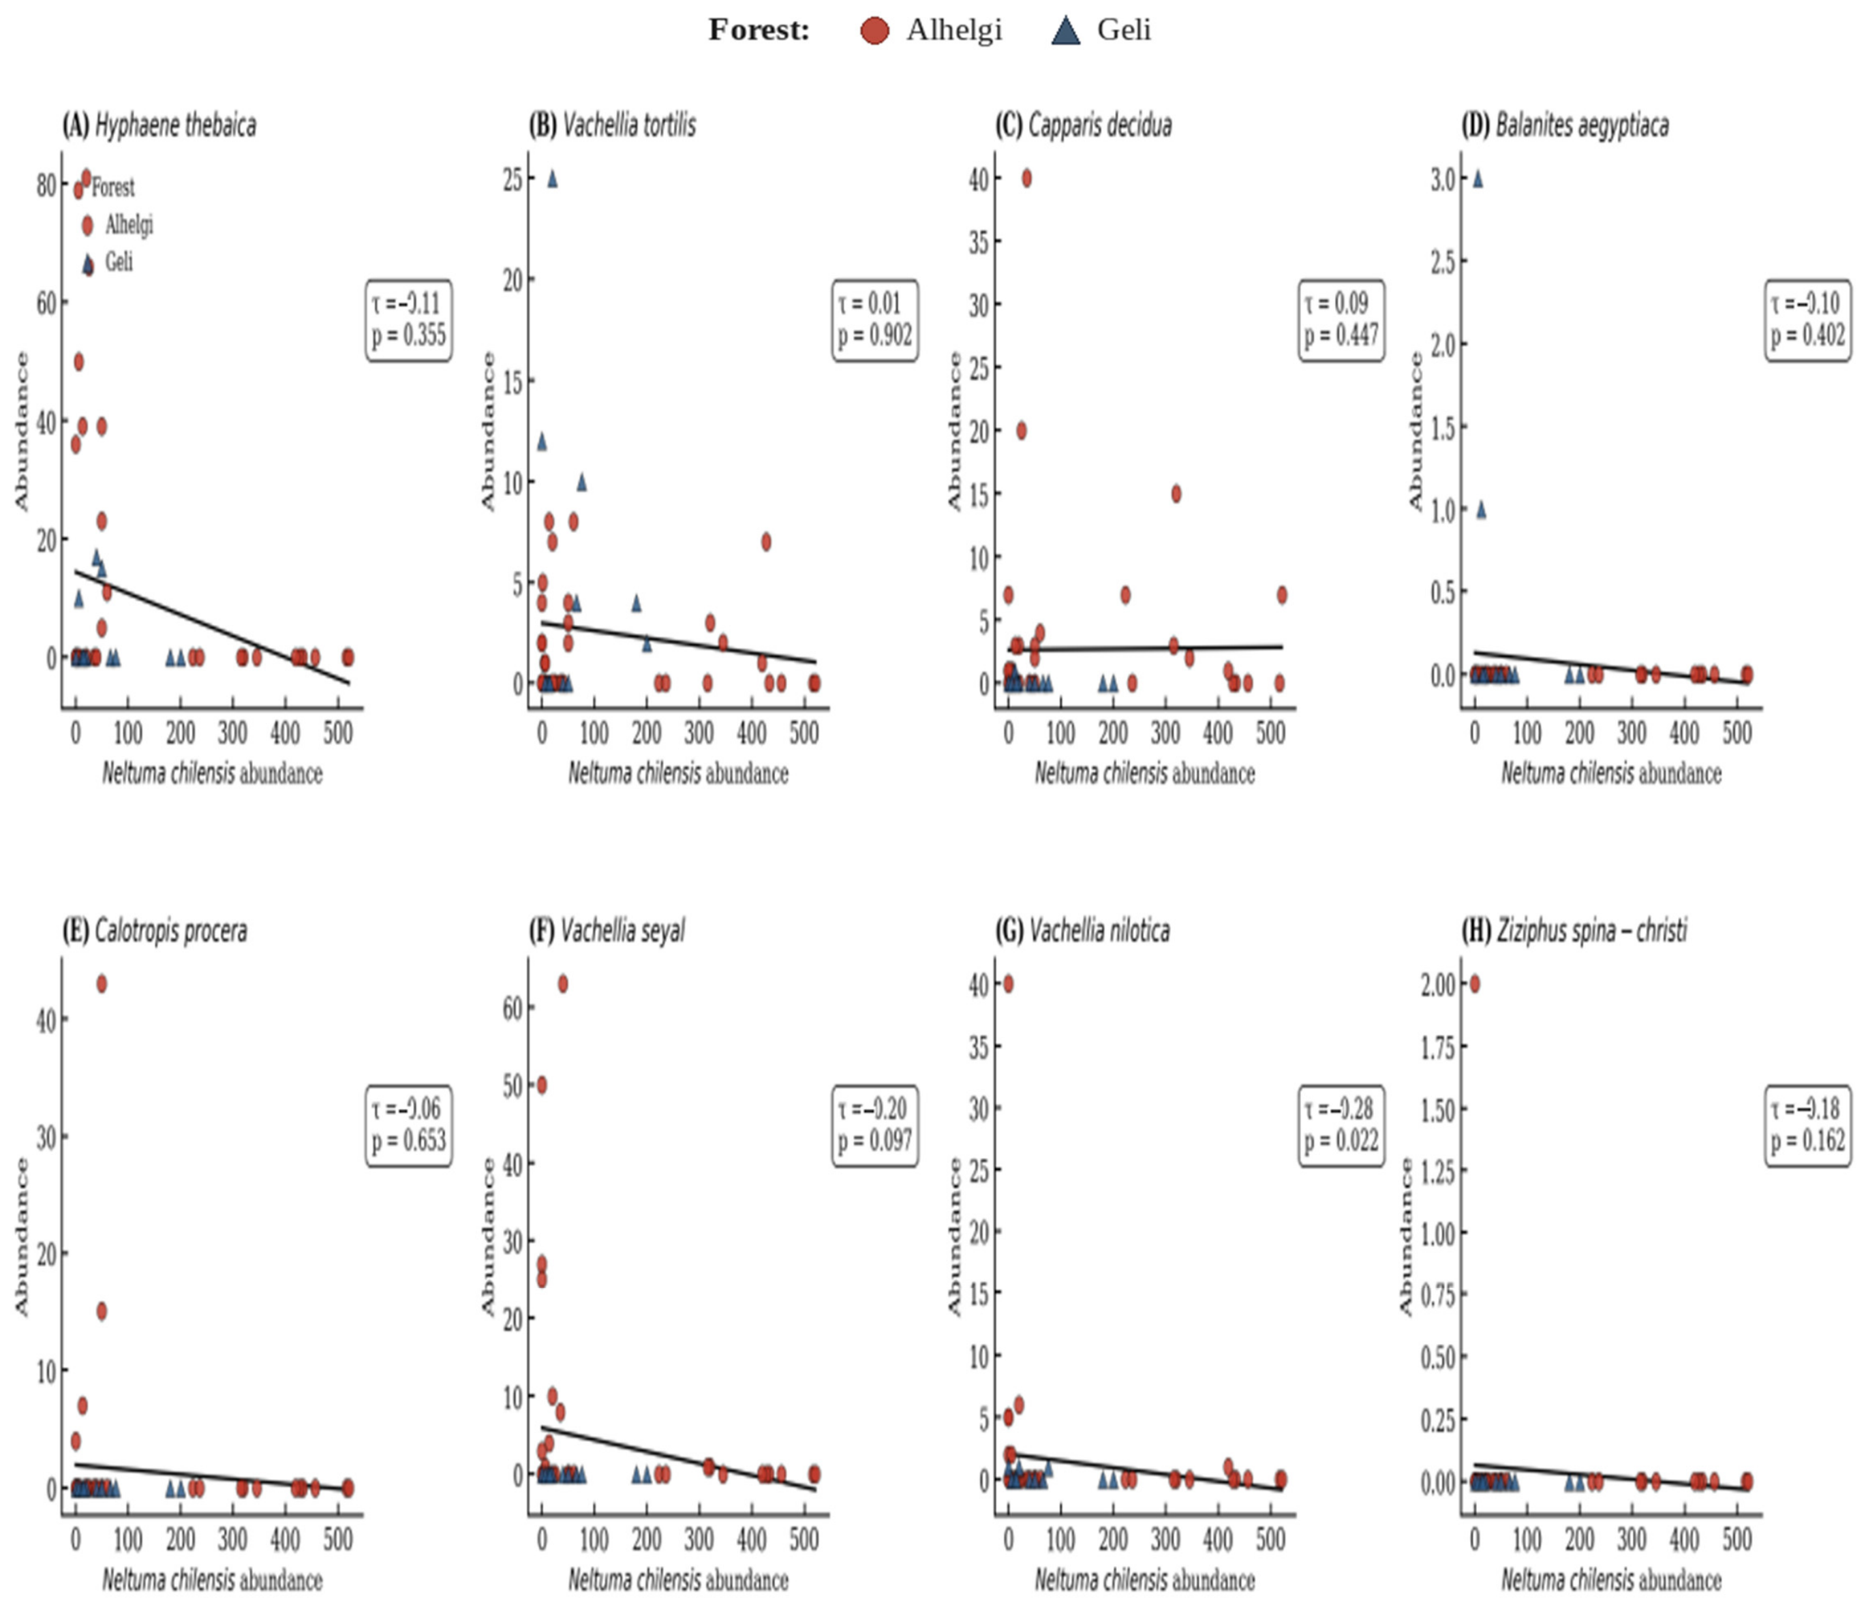
At the individual species level, Kendall’s tau (τ) correlation analysis was used to examine the relationship between N. chilensis abundance and the abundance of native species. A statistically significant negative association was observed only for Vachellia nilotica (Figure 6G; τ = −0.28, p = 0.022), indicating that higher N. chilensis abundance was associated with reduced abundance of this species. In contrast, Vachellia tortilis and Capparis decidua (Figure 6B,C) showed no significant relationship with N. chilensis abundance (τ = 0.014, p = 0.902 and τ = 0.09, p = 0.447, respectively). The result suggests that its abundance was largely unaffected by the invasion. Similarly, H. thebaica (Doum palm), an ecologically important native species, exhibited a weak negative association with N. chilensis abundance (Figure 6A; τ = − 0.11, p = 0.355); however, this relationship was not statistically significant. Likewise, no statistically significant associations were detected between N. chilensis abundance and the abundance of the remaining native species, indicating that, individually, these species showed no measurable response to increasing invasion intensity under the conditions of this study.

4. Discussion

4.1. Ecological Dominance of N. chilensis and Its Effects on Forest Composition and Structure

The findings indicate that N. chilensis has attained strong ecological dominance in the Alhelgi and Geli forests (Table 2), as evidenced by its exceptionally high density and Importance Value Index (IVI), accounting for 58%–66% of the total IVI (175 and 197 out of 300, respectively). Such dominance represents an unusually high level of structural dominance that is rarely observed among native species under natural conditions. This overwhelming dominance was accompanied by a marked decline in native vegetation, with the density of H. thebaica decreasing by 73%–91% relative to its abundance in the uninvaded Um Bashim forest. These changes indicate a substantial shift in vegetation composition and forest structure, suggesting that N. chilensis is progressively displacing native wood species and altering ecosystem functioning. Such invasion patterns are consistent with previous studies reporting that Neltuma species commonly establish dense monospecific stands that suppress native vegetation, reduce species richness, and disrupt ecological processes in dryland ecosystems [2,5,8,28]. The strong competitive capacity of N. chilensis, coupled with its rapid growth, deep rooting system, drought tolerance, and nitrogen-fixing ability, is likely to enhance its ecological persistence and facilitates its widespread expansion. Therefore, continued invasion may lead to long-term degradation of native forest structure, reduced regeneration potential of indigenous species, and declining ecosystem resilience. In contrast, Um Bashim Forest, where N. chilensis is absent, is dominated by H. thebaica, suggesting that native species can maintain structural stability in the absence of invasive pressure. This highlights the critical role of invasion in compositional changes and is consistent with the strong competitive effects of N. chilensis, similar findings have been reported in semi-arid ecosystems, where invasive wood species significantly alter stand structure and reduce native species abundance [6,28,29], as well as modify soil stability, increase erosion, and reshape plant community structure [7]. Changes in species composition and structures provide a more inclusive comprehension of invasion impacts than species count alone. Invasive species can alter community composition by replacing native species, modifying vegetation structure, suppressing natural regeneration, and disrupting key ecosystem functions [3,30]. Therefore, evaluating species composition, structural attributes, and ecosystem function is essential for accurately assessing the ecological impacts of biological invasions.
The increased dominance of Fabaceae in invaded forests was primarily driven by the proliferation of Neltuma chilensis. This pattern may reflect potential competition with native leguminous species sharing similar ecological requirements, although species-specific replacement was not directly assessed. Therefore, these family-level shifts should be interpreted cautiously, as they may largely reflect the dominance of a single invasive species rather than a uniform response across Fabaceae.

4.2. Impact of N. chilensis Invasion on Species Richness and Native Species Abundance

Neltuma species have been shown to be aggressive invaders that displace native species through competition and alter ecosystems, making them unsuitable habitats for native species, thereby causing obvious reductions in species richness, particularly among woody species [12]. The abundance of N. chilensis was identified as the second most important determinant influencing ecosystem impacts, consistent with evidence that the ecological effects of invasive species generally increase with their abundance [9]. This species rapidly dominates colonized areas due to its strong competitive ability, enabling it to effectively compete for light, water, nutrients, and space. Invasive success is further enhanced by its nitrogen-fixing capacity, which improves soil nutrient availability and facilitates establishment, persistence, and spread of the species [12,31]. In addition, its aggressive seeds dispersal mechanism and high pod production, mature trees producing approximately 90–140 kg of pods per season, contribute significantly to its rapid expansion and colonization potential [12].
The findings of this study (Figure 4) indicate that increasing abundance of N. chilensis is significantly associated with declines in species richness and native species abundance at the community level (Figure 5). These results suggest that N. chilensis invasion alters the composition and structure of the plant community, thereby reducing native biodiversity. The competitive advantages of N. chilensis, including rapid growth, an extensive root system, and high drought tolerance, enable it to outcompete native vegetation and suppress regeneration processes [5,8].
These findings are consistent with studies demonstrating that invasive wood species can substantially reduce the abundance, diversity, and regeneration potential of native species in dryland ecosystems [6,10], thereby disrupting nutrient cycling, reducing forest productivity, and threatening the persistence of native vegetation [3,10]. In Afar region, Ethiopia, N. juliflora invasion reduced species richness and diversity [32]. In Namibia, Prosopis spp. had largely replaced the natural vegetation such as native species, shrubs and herbaceous plants [33]. Similarly, in North Cape, South Africa, N. velutina invasion has significantly decrease in native species, density, and richness [2,34]. In addition, the allelopathic effects of Prosopis species may further suppress the germination and growth of native species [35]. Collectively, these findings suggest that N. chilensis invasion poses a serious ecological threat to sustainability, structural stability, biodiversity, and functional integrity of H. thebaica forest ecosystems.
Overall, the analysis indicated that increasing abundance of N. chilensis was associated with a general decline in the abundance of native woody species at the community level. However, species-specific analyses revealed that these negative relationships were not statistically significant for most native species (Figure 6). The only exception was Vachellia nilotica, which exhibited a significant negative association with N. chilensis abundance (Figure 6G; τ = −0.28, p = 0.022). These findings suggest that the ecological impacts of N. chilensis invasion are more pronounced at the community level than at the level of individual species. The absence of statistically significant responses for most native species should not be interpreted as evidence of negligible ecological effects. Rather, it likely reflects interspecific variation in ecological tolerance, competitive ability, regeneration strategies, and spatial distribution, resulting in differential responses to invasion.
Although no significant relationships were detected between N. chilensis abundance and the abundance of Vachellia tortilis (Figure 6B; τ = 0.014, p = 0.902), Capparis decidua (Figure 6C; τ = 0.09, p = 0.447), or Hyphaene thebaica (Figure 6A; τ = − 0.11, p = 0.355), these findings do not exclude long-term ecological consequences. H. thebaica, an ecologically important native species, exhibited a weak negative association with N. chilensis abundance. Continued expansion of N. chilensis may therefore pose a long-term threat to the persistence of this species by reducing regeneration and recruitment, particularly in heavily invaded areas where competitive pressures are greatest.
Invasive woody species can exert cumulative impacts on ecosystem structure and community composition long before detectable declines occur in populations of individual species [3,36]. In dryland ecosystems, invasion impacts may therefore emerge more clearly through reductions in overall native abundance, and regeneration potential rather than through uniform responses of single species. Furthermore, the significant decline observed for Vachellia nilotica suggests that some native species are particularly vulnerable to competition from Neltuma chilensis. According to Niche Theory, species exhibiting greater overlap in resource requirements with invasive species are expected to experience stronger competitive effects through competition for limiting resources such as light, water, and nutrients [37,38]. The rapid growth, deep rooting system, drought tolerance, nitrogen-fixing capacity, and potential allelopathic effects of N. chilensis may therefore intensify resource limitation for sensitive native species [5,35]. The stronger response of V. nilotica suggests that this species may experience greater niche overlap with N. chilensis or possess lower tolerance to invasion-related resource competition than the other native woody species examined in this study. In Sudan, V. nilotica is a characteristic component of riverine and floodplain vegetation, where relatively high soil moisture and periodic flooding promote seedling establishment and regeneration. Recent studies from Sudanese riverine forests have shown vigorous regeneration of V. nilotica in highly flooded sites, reflecting the species’ close association with moist riparian habitats [39].
Such habitats may be particularly susceptible to invasion, potentially increasing niche overlaps and competitive interactions between V. nilotica and N. chilensis. By contrast, the absence of statistically significant responses in the other native woody species may reflect differences in ecological tolerance, phenotypic plasticity, or resource-use strategies that reduce their susceptibility to invasion impacts [37]. However, these non-significant relationships should be interpreted cautiously, as limited sample size and natural environmental variability may have reduced the statistical power to detect subtle ecological effects [40,41]. Similar studies have shown that Prosopis invasions affect native species unevenly, depending on their ecological characteristics and competitive abilities [8].
Therefore, these findings indicate that N. chilensis invasion is driving gradual changes in the composition and structure of native woody species communities, with the magnitude of species-specific impacts depending on differences in ecological sensitivity, competitive interactions, and adaptive capacity.

4.3. Study Limitations

This study has several limitations. First, the observational and cross-sectional design limits causal inference; therefore, the observed associations between N. chilensis abundance and native species richness or abundance should not be interpreted as definitive evidence of causation. Second, the study was conducted in three forest reserves within one locality, which may limit generalization to other Doum palm forests in Sudan. Long-term monitoring, repeated vegetation inventories, and experimental or quasi-experimental studies are recommended to evaluate temporal trends, recruitment and mortality, and the mechanisms underlying the observed invasion effects.

4.4. Management Implications

The findings indicate that the degradation of H. thebaica (Doum palm) forests is closely linked to the ecological dominance of N. chilensis, particularly in the Alhelgi and Geli forests, where the invasive species has substantially displaced native vegetation and altered forest structure. These findings underscore the need for targeted management strategies to limit further invasion and support the recovery of native woody species. Priority interventions should include the control of N. chilensis in invaded forests, restoration of native vegetation, particularly H. thebaica and Vachellia nilotica, and continued ecological monitoring to track invasion progression across the studied forests. Such measures are essential for maintaining the structural integrity, species richness, and long-term ecological resilience of H. thebaica (Doum palm) forests in dryland Sudan.

5. Conclusions

This study indicates that N. chilensis is strongly associated with vegetation change and degradation in H. thebaica (Doum palm) forests. Increasing abundance of N. chilensis was significantly associated with reduced species richness and lower native species abundance at the community level, confirming its strong influence on plant community structure and composition. Although the invasion had no statistically significant effect on most individual native species, except for Vachellia nilotica, it exerted substantial ecological pressure on the broader plant community, resulting in altered ecosystem dynamics and reduced biodiversity. Overall, the study highlights the urgent need for integrated management and conservation strategies that combine invasive species control, restoration of native vegetation, and sustainable forest resource use. Implementing these measures will enhance ecosystem resilience, conserve species richness and abundance, and promote the long-term sustainability of Doum palm forest ecosystems.

Author Contributions

Conceptualization, Methodology, Data Curation, Investigation, Writing—Original Draft: H.A.A.; Data Curation, Formal Analysis, Software, Visualization: A.O.; Supervision, Writing—Review and Editing: A.H.; Supervision, Formal Analysis, Writing—Review and Editing: D.A.M.D.A.A. All authors have read and agreed to the published version of the manuscript.

Funding

A.O. appreciates funding from the Austrian Science Fund FWF (grant DOI https://doi.org/10.55776/ESP5590324). H.A.A was supported by the Ministry of Higher Education and Scientific Research in Sudan. No additional external funding was received.

Institutional Review Board Statement

Not applicable. This study involved ecological field surveys and vegetation inventories and did not involve human participants or animal subjects.

Data Availability Statement

The data will be available from the corresponding author upon reasonable request.

Acknowledgments

The authors gratefully acknowledge the Ministry of Higher Education and Scientific Research of Sudan and University of Gezira for their support. Warm thanks to the Austrian Science Fund FWF (grant DOI https://doi.org/10.55776/ESP5590324). Special thanks are given to University of Sopron for hosting and supervision.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Catford, J.A.; Vesk, P.A.; Richardson, D.M.; Pyšek, P. Quantifying levels of biological invasion: Towards the objective classification of invaded and invasible ecosystems. Glob. Change Biol. 2012, 18, 44–62. [Google Scholar] [CrossRef] [Scilit]
  2. Tiawoun, M.A.P.; Malan, P.W.; Comole, A.A.; Moshobane, M.C. Impact of Prosopis velutina Wooton on the composition and diversity of native woody species in a semi-arid zone along the Molopo River, South Africa. Plants 2023, 12, 1561. [Google Scholar] [CrossRef] [Scilit]
  3. Pyšek, P.; Hulme, P.E.; Simberloff, D.; Bacher, S.; Blackburn, T.M.; Carlton, J.T.; Dawson, W.; Essl, F.; Foxcroft, L.C.; Genovesi, P.; et al. Scientists’ warning on invasive alien species. Biol. Rev. 2020, 95, 1511–1534. [Google Scholar] [CrossRef] [Scilit]
  4. Roychoudhury, N. Forest invasive species and their management. In Textbook of Forest Science; Springer Nature: Singapore, 2025; pp. 315–331. [Google Scholar] [CrossRef] [Scilit]
  5. Ravhuhali, K.E.; Mudau, H.S.; Moyo, B.; Hawu, O.; Msiza, N.H. Prosopis Species—An Invasive Species and a Potential Source of Browse for Livestock in Semi-Arid Areas of South Africa. Sustainability 2021, 13, 7369. [Google Scholar] [CrossRef] [Scilit]
  6. Ndhlovu, T.; Milton, S.J.; Esler, K.J. Effect of Prosopis (Mesquite) Invasion and Clearing on Vegetation Cover in Semi-Arid Nama Karoo Rangeland, South Africa. Afr. J. Range Forage Sci. 2016, 33, 11–19. [Google Scholar] [CrossRef] [Scilit]
  7. Powell, K.I.; Chase, J.M.; Knight, T.M. A Synthesis of Plant Invasion Effects on Biodiversity across Spatial Scales. Am. J. Bot. 2011, 98, 539–548. [Google Scholar] [CrossRef] [Scilit]
  8. Shiferaw, H.; Dzikiti, S.; Schaffner, U.; van Wilgen, B.W. The Impacts of Invading Prosopis Trees on Water Resources. In The Ecology and Management of Invasive Prosopis Trees in Eastern Africa; CABI: Wallingford, UK, 2024; pp. 94–107. [Google Scholar] [CrossRef] [Scilit]
  9. Bradley, B.A.; Laginhas, B.B.; Whitlock, R.; Allen, J.M.; Bates, A.E.; Bernatchez, G.; Diez, J.M.; Early, R.; Lenoir, J.; Vilà, M.; et al. Disentangling the Abundance-Impact Relationship for Invasive Species. Proc. Natl. Acad. Sci. USA 2019, 116, 9919–9924. [Google Scholar] [CrossRef] [Scilit]
  10. Eshete, A.; Treydte, A.C.; Hailemariam, M.; Solomon, N.; Dejene, T.; Yilma, Z.; Birhane, E. Variations in Soil Properties and Native Woody Plant Species Abundance under Prosopis juliflora Invasion in Afar Grazing Lands, Ethiopia. Ecol. Process. 2020, 9, 36. [Google Scholar] [CrossRef] [Scilit]
  11. Zhu, Y.; Zhang, J.; Zhang, Y.; Qin, S.; Shao, Y.; Gao, Y. Responses of Vegetation to Climatic Variations in the Desert Region of Northern China. Catena 2019, 175, 27–36. [Google Scholar] [CrossRef] [Scilit]
  12. van Wilgen, B.W.; Schaffner, U.; Ehrensperger, A.; Bekele, K. Addressing the Ecology and Management of Prosopis Species in Eastern Africa. In The Ecology and Management of Invasive Prosopis Trees in Eastern Africa; CABI: Wallingford, UK, 2024; pp. 1–13. [Google Scholar] [CrossRef] [Scilit]
  13. Abdel Magid, T.D.; El Siddig, E.N.A.; Ahmed, A.S.; Ahmed, M.T.E. Mesquite in Sudan: A Boon or Bane for Dry Lands? Its Socioeconomic and Management Aspects in Kassala State, Sudan. J. For. Prod. Ind. 2014, 3, 182–190. [Google Scholar]
  14. Babiker, A.G.T.; Nagat, E.M.; Ahmed, E.A.M. Mesquite (Prosopis juliflora): A Threat to Agriculture and Pastoralism in Sudan. In Proceedings of the 2nd International Workshop on Invasive Plants in the Mediterranean Type Regions of the World, Trabzon, Turkey, 2–6 August 2010; pp. 283–287. [Google Scholar]
  15. Shackleton, R.T.; Le Maitre, D.C.; Pasiecznik, N.M.; Richardson, D.M. Prosopis: A Global Assessment of the Biogeography, Benefits, Impacts and Management of One of the World’s Worst Woody Invasive Plant Taxa. AoB Plants 2014, 6, plu027. [Google Scholar] [CrossRef] [Scilit]
  16. Abass, R.S.E.B.; Abd Alla, M.Y.M.; El-Eragi, A.M.E.H. Spatial Risk Analysis of Water Borne Diseases (Bovine Leptospirosis) in the River Nile State-Sudan. J. Geogr. Inf. Syst. 2014, 6, 1–10. [Google Scholar] [CrossRef]
  17. Abdelkarim, H.A.; Ahmed, D.A.M.; Yagoub, Y.E.; Siddig, A.A. Composition, Structure and Regeneration Status of Hyphaene thebaica (L.) Mart. Natural Forests in Dry Lands of Sudan. Agric. For. J. 2021, 5, 82–88. [Google Scholar]
  18. Dafa-Alla, D.A.M.; Abdelkarim, H.A.; Abu Elbashar, A.I.; Hassan, M.H. Boswellia papyrifera, a tree of economic importance in dryland Sudan: Dendrometric parameters and tapping characteristics. Asian J. For. 2023, 7, 10–16. [Google Scholar] [CrossRef] [Scilit]
  19. Darbyshire, I.; Kordofani, M.; Farag, I.; Candiga, R.; Pickering, H. (Eds.) The Plants of Sudan and South Sudan: An Annotated Checklist; Kew Publishing, Royal Botanic Gardens, Kew: Richmond, UK, 2015; 400p, ISBN 978-1-84246-473-1. [Google Scholar]
  20. Dafa-Alla, D.A.M.; Gibreel, H.H.; Siddig, A.A.; Yagoub, Y.E.; Abdelkarim, H.A.; Saeed, K.H.; Abuelbashar, A.I. Exploring trees diversity and ecological value of mountain forests in the Blue Nile Region of Sudan. Open J. Ecol. 2024, 14, 245–256. [Google Scholar] [CrossRef]
  21. POWO. Plants of the World Online. Available online: https://powo.science.kew.org/ (accessed on 2 September 2026).
  22. WFO. World Flora Online. Available online: http://www.worldfloraonline.org/ (accessed on 2 September 2026).
  23. Hughes, C.E.; Ringelberg, J.J.; Lewis, G.P.; Catalano, S.A. Disintegration of the genus Prosopis L. (Leguminosae, Caesalpinioideae, mimosoid clade). PhytoKeys 2022, 205, 147–189. [Google Scholar] [CrossRef] [Scilit]
  24. Aye, T.H.; Shibata, S. Vegetation Structure and Tree Species Diversity inside and outside a Newly Established Zalon Taung National Park in Northwest Myanmar. Int. J. For. Res. 2023, 2023, 8409374. [Google Scholar] [CrossRef] [Scilit]
  25. Dessie, Y.; Amsalu, N.; Awoke, B.; Gebeyehu, G. Floral diversity, structural integrity, and regeneration patterns of Endba-Zend dry Afromontane Forest in Northwestern Ethiopia. BMC Ecol. Evol. 2025, 25, 49. [Google Scholar] [CrossRef] [Scilit]
  26. Mohammed, E.M.; Hamid, E.A.; Ndakidemi, P.A.; Treydte, A.C. The stocking density and regeneration status of Balanites aegyptiaca in Dinder Biosphere Reserve, Sudan. Trees For. People 2022, 8, 100259. [Google Scholar] [CrossRef] [Scilit]
  27. Mohammed, E.M.; Yasin, E.H.; Mulyana, B. Analysis of species richness variability, spatial distribution, and carbon stock in Okalma Natural Forest Reserve, Sudan. Anthr. Sci. 2025, 4, 30–41. [Google Scholar] [CrossRef] [Scilit]
  28. Simberloff, D.; Martin, J.L.; Genovesi, P.; Maris, V.; Wardle, D.A.; Aronson, J.; Courchamp, F.; Galil, B.; García-Berthou, E.; Pascal, M.; et al. Impacts of biological invasions: What’s what and the way forward. Trends Ecol. Evol. 2013, 28, 58–66. [Google Scholar] [CrossRef] [Scilit]
  29. Mayfield, A.E., III; Seybold, S.J.; Haag, W.R.; Johnson, M.T.; Kerns, B.K.; Kilgo, J.C.; Larkin, D.J.; Lucardi, R.D.; Moltzan, B.D.; Pearson, D.E.; et al. Impacts of invasive species in terrestrial and aquatic systems in the United States. In Invasive Species in Forests and Rangelands of the United States; Springer: Cham, Switzerland, 2021; pp. 5–39. [Google Scholar] [CrossRef] [Scilit]
  30. Vilà, M.; Espinar, J.L.; Hejda, M.; Hulme, P.E.; Jarošík, V.; Maron, J.L.; Pergl, J.; Schaffner, U.; Sun, Y.; Pyšek, P. Ecological impacts of invasive alien plants: A meta-analysis of their effects on species, communities and ecosystems. Ecol. Lett. 2011, 14, 702–708. [Google Scholar] [CrossRef] [Scilit]
  31. Ansley, R.J.; Cooper, C.; Zhang, T. Invasion promotes invasion: Facilitation of C3 perennial grass dominance in mixed C3/C4 grassland by an invasive C3 woody sprouter (Prosopis glandulosa). Ecol. Evol. 2019, 9, 13438–13449. [Google Scholar] [CrossRef] [Scilit]
  32. Linders, T.E.W.; Schaffner, U.; Eschen, R.; Abebe, A.; Choge, S.K.; Nigatu, L.; Mbaabu, P.R.; Shiferaw, H.; Allan, E. Direct and indirect effects of invasive species: Biodiversity loss is a major mechanism by which an invasive tree affects ecosystem functioning. J. Ecol. 2019, 107, 2660–2672. [Google Scholar] [CrossRef] [Scilit]
  33. Shiferaw, H.; Bewket, W.; Eckert, S. Performances of machine learning algorithms for mapping fractional cover of an invasive plant species in a dryland ecosystem. Ecol. Evol. 2019, 9, 2562–2574. [Google Scholar] [CrossRef] [Scilit]
  34. Strohbach, B.J.; Ntesa, C.; Kabajani, M.; Shidolo, E.K.; d’Alton, C.D. Prosopis encroachment along the Fish River at Gibeon, Namibia: Habitat preferences, population densities and the effect on the environment. Dinteria 2015, 35, 53–73. [Google Scholar]
  35. Getachew, S.; Demissew, S.; Woldemariam, T. Allelopathic effects of the invasive Prosopis juliflora (Sw.) DC. on selected native plant species in Middle Awash, Southern Afar Rift of Ethiopia. Manag. Biol. Invasions 2012, 3, 105–114. [Google Scholar] [CrossRef] [Scilit]
  36. Abdella, U.; Desta, A.B.; Berhanu, Y. Richness and abundance of invasive and expansive plant species and their associated effects on native vegetation in a semi-arid rangeland of the Rift Valley. Glob. Ecol. Conserv. 2025, 60, e03602. [Google Scholar] [CrossRef] [Scilit]
  37. Gioria, M.; Osborne, B.A. Resource competition in plant invasions: Emerging patterns and research needs. Front. Plant Sci. 2014, 5, 501. [Google Scholar] [CrossRef] [Scilit]
  38. Dubart, M.; Pantel, J.H.; Pointier, J.-P.; Jarne, P.; David, P. Modeling competition, niche, and coexistence between an invasive and a native species in a two-species metapopulation. Ecology 2019, 100, e02700. [Google Scholar] [CrossRef] [Scilit]
  39. Mohammed, E.M.I.; Hagr, E.A.A.; Ahmed, A.K.M.; Harouna, D.V. Immersion effects and flooding susceptibility index for Vachellia nilotica trees in Remaila Riverine Reserved Forest, Sudan. J. Arid Environ. 2026, 235, 105559. [Google Scholar] [CrossRef] [Scilit]
  40. Nakagawa, S.; Cuthill, I.C. Effect size, confidence interval and statistical significance: A practical guide for biologists. Biol. Rev. 2007, 82, 591–605. [Google Scholar] [CrossRef] [Scilit]
  41. Button, K.S.; Ioannidis, J.P.A.; Mokrysz, C.; Nosek, B.A.; Flint, J.; Robinson, E.S.J.; Munafò, M.R. Power failure: Why small sample size undermines the reliability of neuroscience. Nat. Rev. Neurosci. 2013, 14, 365–376. [Google Scholar] [CrossRef] [Scilit]
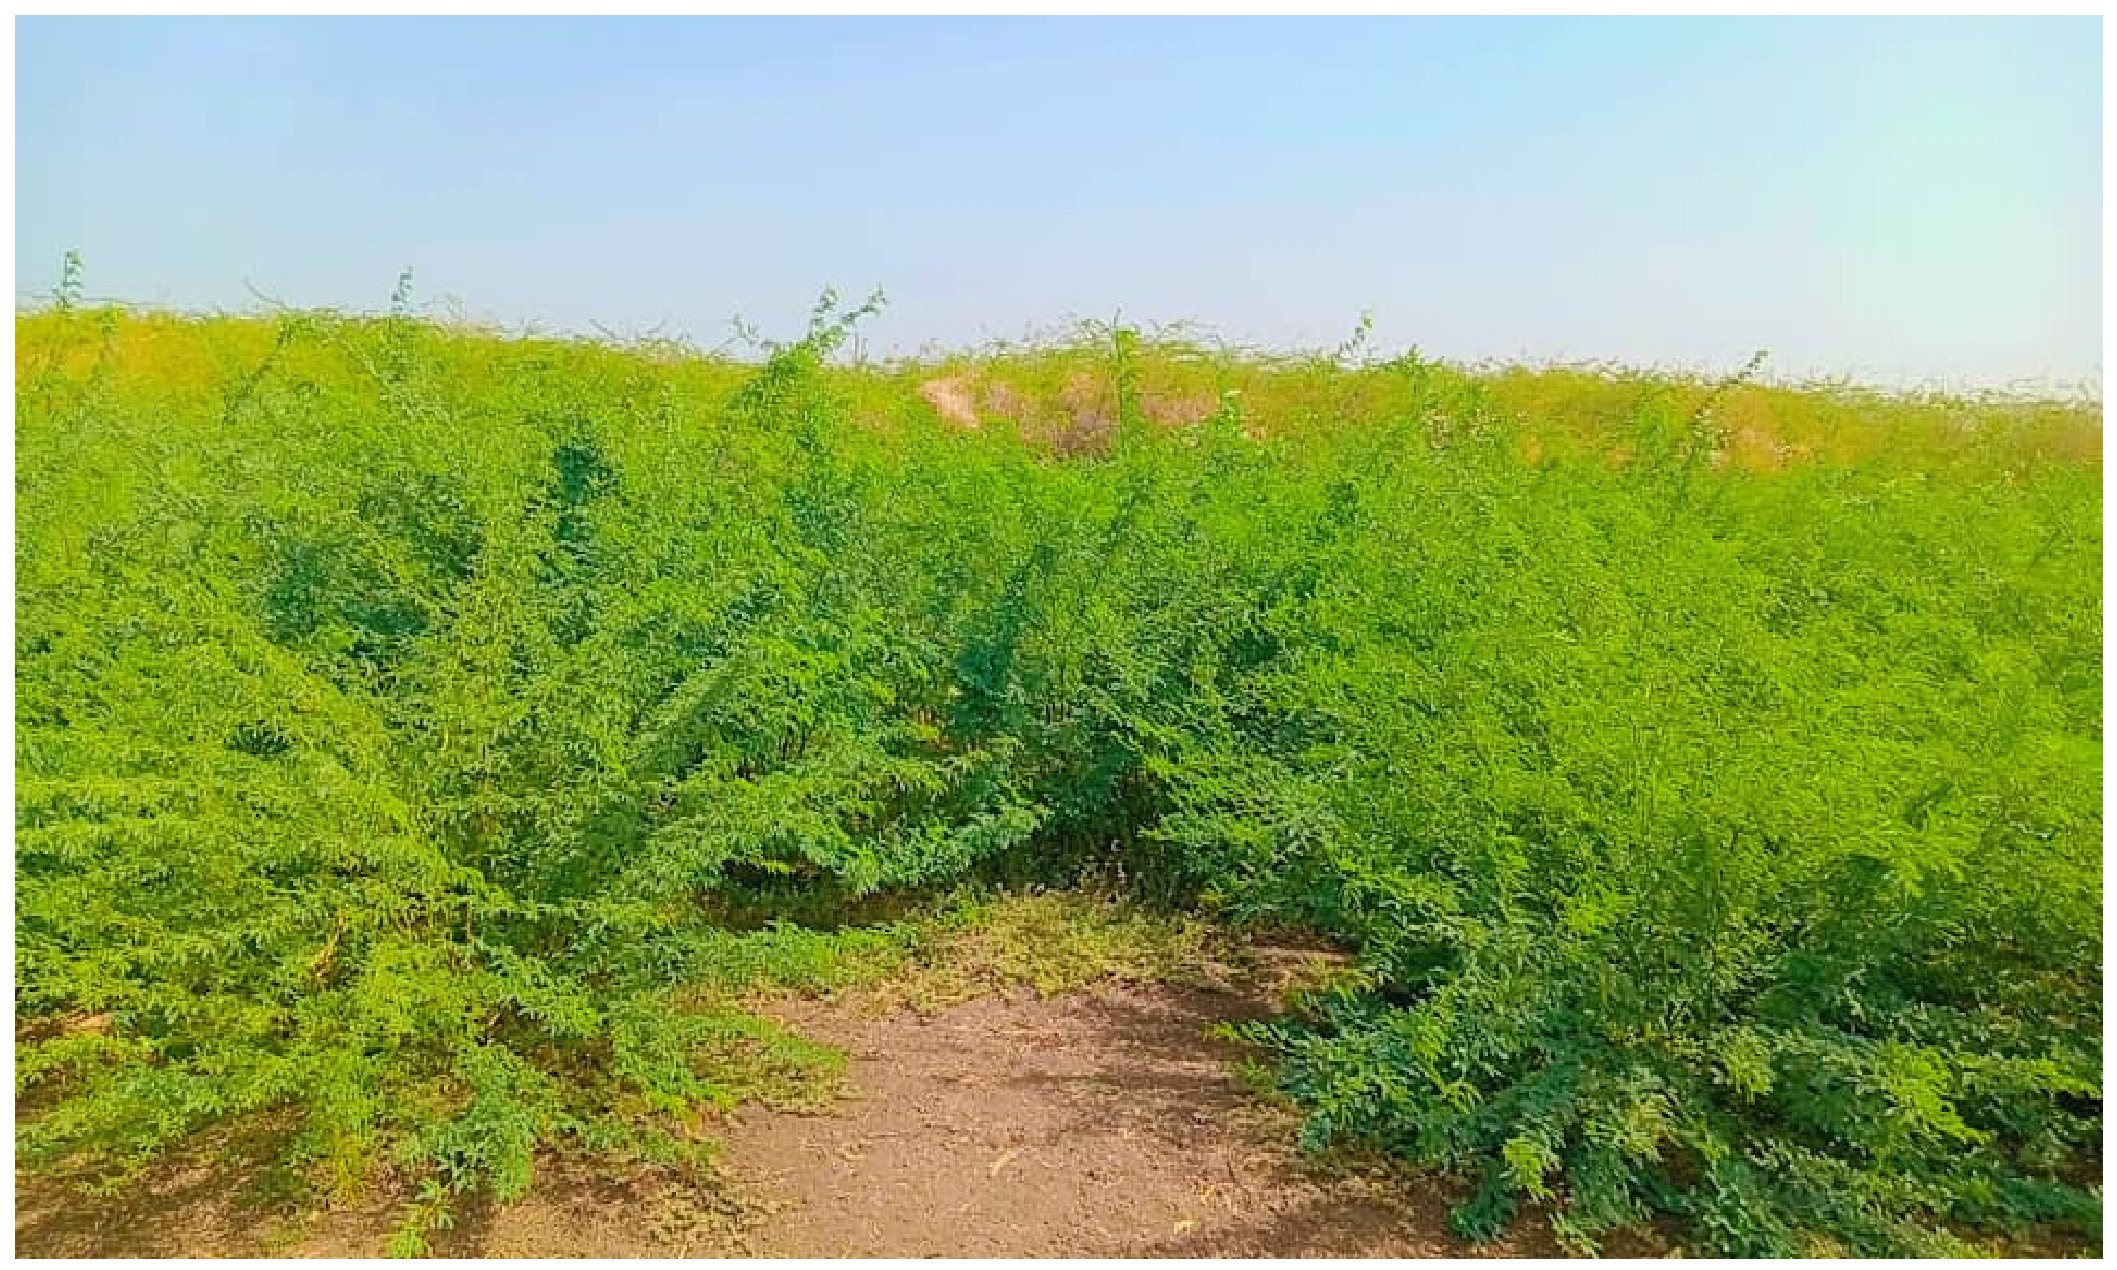
Figure 1. N. chilensis invasion in the study area. Photograph by the authors.
Forests 17 01150 g001
Figure 2. Map of the study area in El-Damar locality River Nile State, Sudan. Adapted by author.
Forests 17 01150 g002
Figure 3. Relative abundance of plant families, genera, and species recorded in the study area.
Forests 17 01150 g003
Figure 4. Relationship between N. chilensis abundance and native species richness at the community level.
Forests 17 01150 g004
Figure 5. Relationship between N. chilensis abundance and native species abundance at the community level.
Forests 17 01150 g005
Figure 6. Relationships between N. chilensis abundance and abundance of individual native species.
Forests 17 01150 g006
Table 1. Phytosociological parameters (F = Frequency, D = Density, A = Abundance, RF = Relative Frequency, RD = Relative Density RA = Relative Abundance, and S = Species richness).
EquationsReference
Frequency (F) = N u m b e r   o f   s a m p l e   u n i t s   i n   w h i c h   t h e   s p e c i e s   o c c u r s / T o t a l   n u m b e r   o f   s a m p l e   u n i t [24,25]
Relative Frequency (RF) = T r e e   s p e c i e s   f r e q u e n c y / T o t a l   f r e q u e n c y   f o r   a l l   s p e c i e s ×100[24,25]
Density (D) = N u m b e r     o f   i n d i v i d u a l s   o f   s p e c i e s / t o t a l   a r e a   o f   s a m p l e   p l o t [24,25]
Relative Density (RD) =  S p e c i e s   d e n s i t y / T o t a l   d e n s i t y   o f   a l l   s p e c i e s × 100[24,25]
Abundance (A) = T o t a l   n u m b e r   o f   i n d i v i d u a l s   o f   a   s p e c i e s / N u m b e r   o f   p l o t s   i n   w h i c h   t h e   s p e c i e s occurs[27]
Relative Abundance (RA) = T r e e   s p e c i e s   a b u n d a n c e / T o t a l   a b u n d a n c e   o f   a l l   s p e c i e s × 100[27]
IVI = RF + RD + RA[27]
Species richness (S) = Total number of species/sample plot area[26]
Table 2. Tree Species Composition, Vegetation Structure and Phytosociological Parameters in the study area.
SpeciesDensity (Trees ha−1)Frequency (%)AbundanceRD
(%)
RF
(%)
RA
(%)
IVI
Um Bashim Forest
Hyphaene thebaica (Arecaceae) 4548256662347137
Vachellia tortilis (Fabaceae)729181126743
Vachellia nilotica (Fabaceae)75362111101839
Ziziphus spina-christi (Rhamnaceae)363610510824
Balanites aegyptiaca (Zygophyllaceae)22465313420
Calotropis procera (Apocynaceae)14915231317
Capparis decidua (Capparaceae)11363210314
Vachellia seyal (Fabaceae)21810.3516
Geli Forest
Neltuma chilensis (Fabaceae)6059167864071197
Vachellia tortilis (Fabaceae)5255107241042
Hyphaene thebaica (Arecaceae)3827145121532
Vachellia nilotica (Fabaceae)32710.412114
Balanites aegyptiaca (Zygophyllaceae)418218211
Calotropis procera (Apocynaceae)1910.1415
Alhelgi Forest
Neltuma chilensis (Fabaceae)131477170832863175
Hyphaene thebaica (Arecaceae)12329438111634
Vachellia tortilis (Fabaceae)35546220225
Capparis decidua (Capparaceae)553118412722
Vachellia seyal (Fabaceae)1746414722
Calotropis procera (Apocynaceae)20111714612
Vachellia nilotica (Fabaceae)1720917312
Ziziphus spina-christi (Rhamnaceae) 1320.04112
Note: RD = Relative Density; RF = Relative Frequency; RA = Relative Abundance; IVI = Importance Value Indices.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.