


Abstract
Compounds of natural origin, an infinite treasure of bioactive chemical entities, persist as an inexhaustible resource for discovering new medicines. In this review, we summarize the naturally occurring ellagitannins, sanguiins, which are bioactive constituents of various traditional medicinal plants, especially from the Rosaceae family. In-depth studies of sanguiin H-6 as an antimicrobial, antiviral, anticancer, anti-inflammatory, and osteoclastogenesis inhibitory agent have led to potent drug candidates. In addition, recently, virtual screening studies have suggested that sanguiin H-6 might increase resistance toward SARS-CoV-2 in the early stages of infection. Further experimental investigations on ADMET (absorption, distribution, metabolism, excretion, and toxicity) supplemented with molecular docking and molecular dynamics simulation are still needed to fully understand sanguiins’ mechanism of action. In sum, sanguiins appear to be promising compounds for additional studies, especially for their application in therapies for a multitude of common and debilitating ailments.
1. Introduction
Most of the discovered drugs are either drugs of natural origin or synthetic derivatives of natural compounds. Thus, a multidisciplinary approach to drug discovery and molecular diversity from natural product sources needs to be combined to provide the best solution to the problems with drug discovery and development [1,2]. Plants are known to be a rich source of pharmacologically active secondary metabolites divided into structural chemical classes [3,4]. One of the pharmacologically valuable classes of phytoconstituents are ellagitannins (ETs), and belonging to them, sanguiins. ETs, water-soluble phenolics, are esters of hexahydroxydiphenic acid and a polyol, usually β-D-glucose or quinic acid [5,6,7]. ET compounds demonstrate an enormous structural variability connected with various possibilities for the linkage of hexahydroxydiphenic residues with the glucose moiety and particularly by their easy susceptibility to creating dimeric and oligomeric derivatives [8]. The polyphenol-protein system and its interactions may underlie the medicinal properties exhibited by members of the ETs family. Fruits and nuts are rich sources of ellagitannins and are important in the human diet due to their properties as micronutrients [9,10]. Due to the limited bioavailability of ellagitannins, as orally administered and the metabolic chemical changes as a result of their transit through the gastrointestinal tract, comprising of hydrolysis and gut microbiota metabolism, the activity of the produced metabolites also needs to be taken into consideration [3].
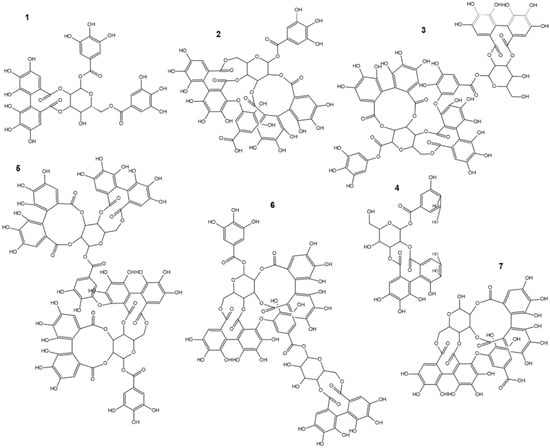
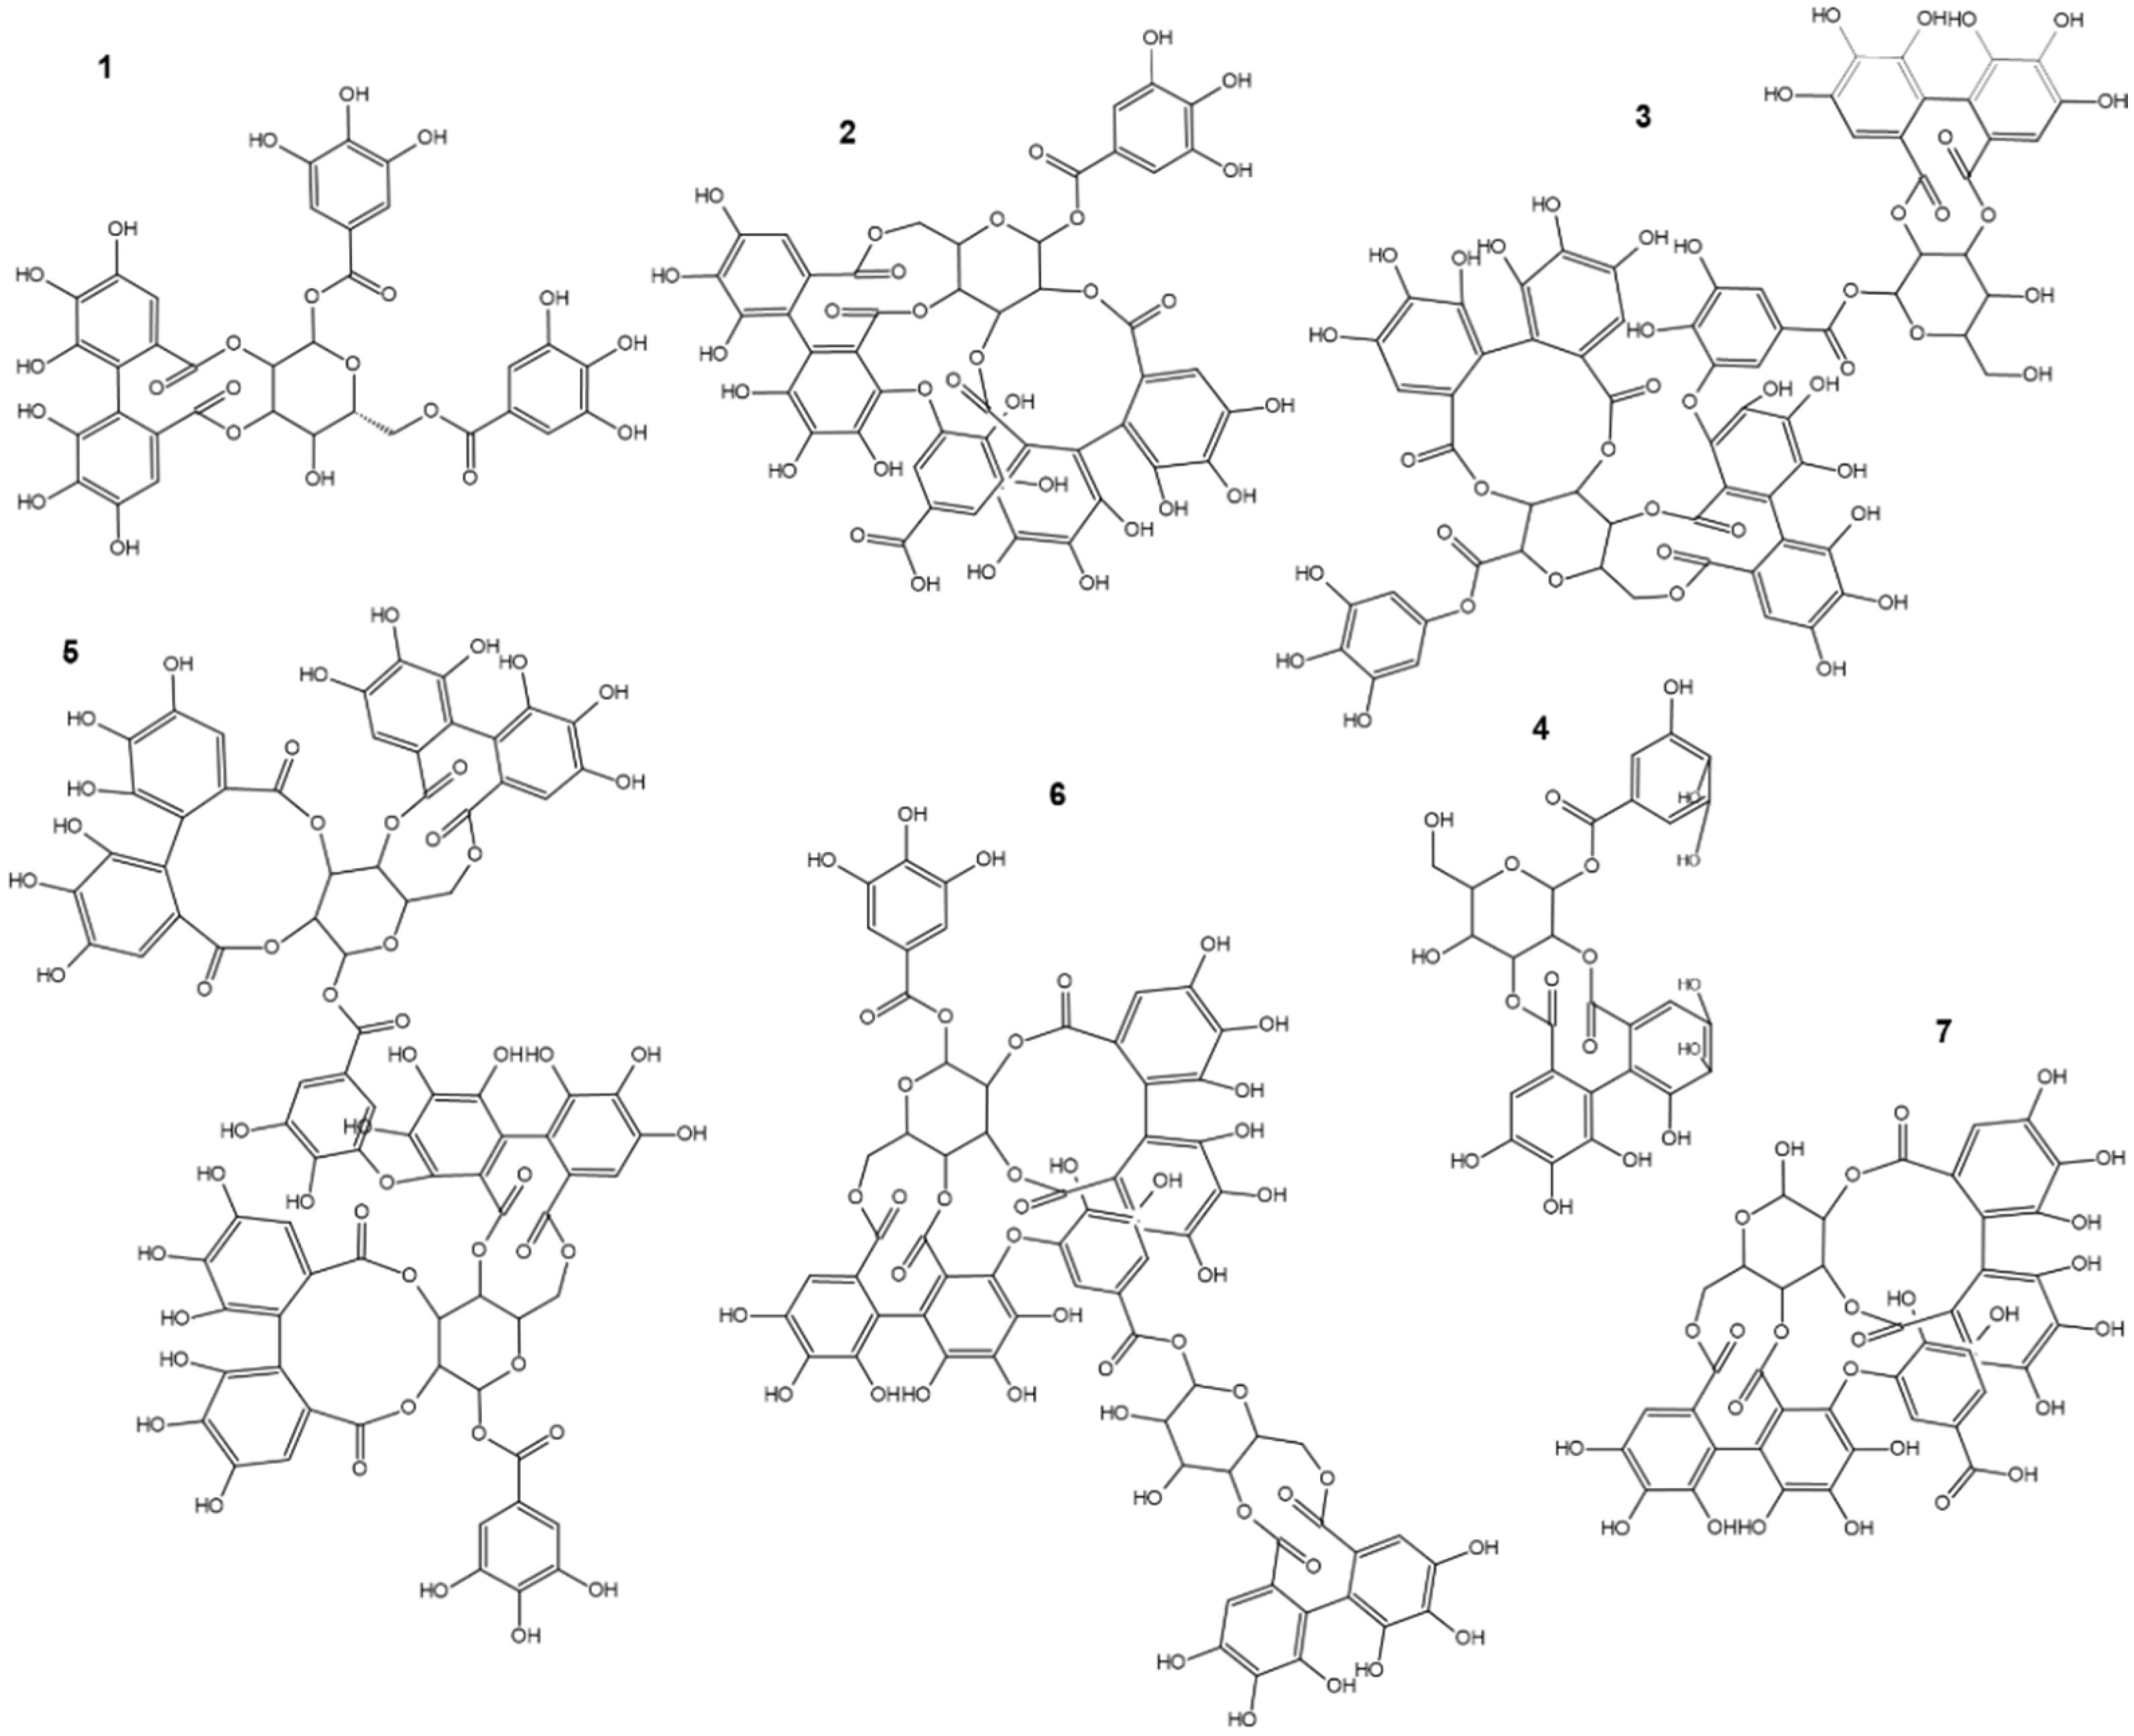
Sanguiins, members of the ET class of hydrolyzable plant polyphenols, are found mainly in the Rosaceae family and are primarily widespread in berries. The main advantage of sanguiins over other common polyphenols in the plant world is their wide distribution in food products. Therefore, their health-promoting properties can be used in a properly balanced diet [11]. In addition to the natural occurrence of sanguiin, there are reports on the synthetic production of sanguiin H-5 [12]. The structural features of sanguiins make them a demanding molecular target. Sanguiin H-1 comprises the characteristic hexahydrodiphenoyl (HHDP) moiety linked with β-D-glucose and 1,6-di-O-galloyl moieties. On the other hand, sanguiin H-2 possesses one galloyl moiety and two sanguisorboyl linking ester groups. Comparing the H-1 and H-4 sanguiins, they differ only in an additional galloyl substituent in sanguiin H-1. The structure of sanguiin H-3, a dimeric ellagitannin, contains two glucose substitutions. Furthermore, the complex structure of sanguiin H-6 includes sanguiin H-2 and pedunculagin moieties. The chemical structure of sanguiin H-10 closely resembles sanguiin H-2, except sanguiin H-10 contains an extra HHDP group. Substitution patterns of sanguiin H-11 also show similarities to sanguiin H-2. The only difference between these structures is the lack of a galloyl moiety in the sanguiin H-11 [13].
Although various bioactivities (e.g., antioxidant, anticancer, antiviral, and antimicrobial) of sanguiins, mainly sanguiin H-6, have been investigated, their pharmacological potential demonstrated in vitro, in silico, and in vivo experimental models has not been clearly organized through review articles. Thus, this manuscript summarizes the findings on the widespread bioactivities of sanguiin H-1 (SH1), sanguiin H-2 (SH2), sanguiin H-3 (SH3), sanguiin H-4 (SH4), sanguiin H-6 (SH6), sanguiin H-10 (SH10), and sanguiin H-11 (SH11) to showcase their potential to be used as therapeutic agents.
2. Methodology
A broad search strategy was used to find English language publications indexed in SCOPUS, PubMed/MEDLINE, Google Scholar, Web of Science (SCI-EXPANDED), Wiley Online Library, Taylor & Francis Online, REAXYS Database, Science Direct/ELSEVIER, and EBSCO Discovery Service (EDS) [14]. These databases were searched systematically for articles published from 1982 to 2021. Relevant publications were selected manually from the following searches: sanguiin, sanguiins, Rosaceae, traditional use, traditional medicine, folk medicine, sanguiin H-6, sanguiin H6, sanguiin H-10, sanguiin H10, sanguiin H-5, sanguiin H5, sanguiin H-2, sanguiin H2, sanguiin H-11, sanguiin H11, sanguiin H-4, sanguiin H4, sanguiin H-3, sanguiin H3, ellagitannins, tannins, Rubus, anticancer, antiviral, SARS-CoV-2, COVID-19, antioxidant, anti-inflammatory, biological activity, antimicrobial, biological potential, metabolism, clinical trials, preclinical trials, chemistry, galloyl moiety, absorption, distribution, excretion, toxicity, perspectives, trials, pharmacological, natural product, secondary metabolites, therapeutic agent, inhibitory activity, inhibitors, dose, efficacy, exposure, experimental model, quantitative analysis, qualitative analysis, geographical location, as well as each of species containing sanguiins combined with traditional use, traditional medicine, or folk medicine. The search terms operated in separate or limited combinations that considered the requirements or limitations of the database being used.
3. Natural Occurrence of Sanguiins
Among various phenolic compounds isolated from the Rosaceae family, tannins and related compounds seem to have a leading position. It is known that plants previously used in folk medicine represent a suitable beginning to discover new potent drugs to treat various human disorders [15]. Sanguiins (Figure 1), naturally occurring ET, have been isolated chiefly from Rubus species and are used as a traditional drug to cure, e.g., diarrhea, menstrual pain, menopause disorders, liver diseases, aphtha, gingivitis, as well as fever, angina, enteritis, hepatitis, concretion, eczema, rheumatism, enterocolitis, bronchitis, prostate disorders, pain, cold, cough, and fever (Table 1) [16,17]. Moreover, SH6 seems to be the most widespread within plants of the Rubus and is present in 22 species of this genus. Furthermore, the largest number of isolated and identified types of sanguiins, including SH2, SH4, SH5, SH6, and SH11, are found in Rubus coreanus [18]. Besides the Rubus genus, sanguiins and their isomers are found and reported in Alchemilla vulgaris, Alchemilla mollis [19], Duchesnea indica [20], Euphorbia fischeriana [21], Fragaria vesca, Fragaria ananassa [22], Punica granatum [23], Terminalia calamansanai [24], as well as in Sanguisorba officinalis [25], and Sanguisorba tenuijolia var. alba [18].
Figure 1.
Sanguiins presented in natural sources. (1) Sanguiin H-1, (2) sanguiin H-2, (3) sanguiin H-3, (4) sanguiin H-4, (5) sanguiin H-6, (6) sanguiin H-10, and (7) sanguiin H-11.
Table 1.
Plants containing sanguiin and its traditional uses.
Among all sanguiins detected in plant material, only part of them was quantitatively analyzed. The place of harvest displays a relevant role in the amount of isolated sanguiins. For example, in Rubus fruticosus fruits, the range of detected SH6 is 135.04–547.48 mg/100 g of d.w. (dry weight) [26] and in Rubus idaeus shoots, 170.9–633.1 mg/100 g of d.w of the extract [27]. Following that, sanguiins content depends on fruits’ ripeness, harvest time, climate, geographic location, and mineral nutrition [10,28]. It is reported that in Rubus and Fragaria species, ellagitannins content represents a range of 50% to 80% of all phenolic compounds [10,29]. In this review, the list of plants that produce sanguiins and their reported traditional uses are tabulated in Table 1.
4. Chromatographic Techniques for the Analysis of Sanguiins
Chromatography displays a crucial role in the analysis of chemical compound mixtures. As a method for the separation and analysis of extracts and fractions from plants, it provides the possibility of qualitative and quantitative determination of the test substance with high resolution [67]. Chromatographic techniques and analysis conditions for detection, quantitative determination, and isolation of sanguiins and their isomers are given in Table 2.
Table 2.
Chromatographic techniques for the analysis of sanguiins.
5. Biological Potential of Sanguiins
Sanguiins, as one of the subgroups of polyphenolic ellagitannins, exhibit various pharmacological activities due to having different chemical structures. They possess a broad spectrum of pharmacological features such as anticancer, anti-inflammatory, antioxidant, osteoprotective, estrogenic, antibacterial, antifungal, and antiviral (including SARS-CoV-2), as shown in Table 3. Various in vivo and in vitro investigations on sanguiins, especially on sanguiin H-6, have elucidated their medicinal characteristics and mechanisms of action [68,69].
Table 3.
Bioactivities of sanguiins reported in in vitro and in vivo experimental models.
5.1. Antioxidant and Anti-Inflammatory Activities
One of the best-shown properties of polyphenols, and following that, sanguiins, is the potential antioxidant effect. Most references mention sanguiin H-6 as the primary compound having antioxidant activity, e.g., its influences on stress and oxidative damage were investigated. The production of peroxynitrite (ONOO-) was induced by the administration of lipopolysaccharide (LPS), followed by the induction of ischemia and reperfusion [88]. It was revealed that receiving SH6 before induction of oxidative damage could reduce the adverse effects associated with the release of ONOO- and enhance the improvement of injured kidney function [72]. Another chemical compound belonging to the sanguiins group that exhibits antioxidant activity is SH11. An examination of the protective effect of SH11 isolated from Sanguisorbae radix and its mechanism against glutamate-induced death in HT22 murine hippocampal cells exposed a significant reduction in glutamine-induced reactive oxygen radicals’ accumulation and calcium ion influx [74]. Furthermore, ellagitannins from the berries of the Rubus family, including dimeric SH6 and SH10, function both as radical scavengers (in a DPPH test) and as antioxidants toward lipid oxidation in food emulsions (studied in bulk and emulsified methyl linoleate, in human low-density lipoprotein in vitro) [75]. The impact of sanguiins on the inflammation process was investigated by measuring their effect on rat neutrophils’ chemotaxis. SH11 and SH6 effectively inhibited the cytokine-induced neutrophil chemoattractant migration process by 10.7% and 33%, respectively, in comparison with the control. Additionally, the study showed no toxic effect of sanguiin on neutrophils [70]. Furthermore, at a concentration of 2.5 μM, SH6 completely inhibited the release of IL-8 induced by tumor necrosis factor α and interleukin-1β and inhibited TNFα stimulated NF-κB transcription [71]. SH6 caused a concentration-dependent reduction in nitrite production, regression in induced NO synthase (iNOS) activity, and an increase in cell viability. Moreover, SH6 showed an apparent scavenging effect for NO generated from sodium nitroprusside (NO donor) [76].
5.2. Osteoclastogenesis Inhibitory Activity
In a subsequent in vitro study, the action of Rubus parvifolius L. and its main component, SH6, was tested as the inhibitor of osteoclastogenesis and bone resorption. Sanguiin influence was based on the reduction in osteoclast differentiation and bone resorption, a decrease in the production of reactive oxygen species, as well as the inhibition of the nuclear translocation of the nuclear factor of activated T cells cytoplasmic-1 (NFATc1), c-Fos, and nuclear factor-κB. Additionally, sanguiin reduced the levels of NFATc1, cathepsin K, c-Src, and inhibited in vivo TNF-α-mediated osteoclastogenesis [47].
5.3. Antibacterial Activity
The growing resistance of bacteria to currently used antibiotics is a growing problem in current medicine [89]. Increasingly emerging research on sanguine antibacterial properties gives hope for the discovery of antibacterial agents with the lack of unpleasant side effects. Examination of the antibacterial activity of fruits of selected Rubus species and compounds (SH6 and ellagic acid) against selected Gram-negative and Gram-positive bacteria allowed assessment of their usefulness in the fight against microorganisms. The results showed that SH6 was active against Streptococcus A (MIC = 0.5 mg/mL), Streptococcus pneumoniae (MIC = 0.5 mg/mL), Corynebacterium diphtheriae (MIC = 0.03 mg/mL), Bacillus subtilis (MIC = 0.5 mg/mL), Clostridium sporogenes (MIC = 0.06 mg/mL), Staphylococcus aureus (MIC = 0.25 mg/mL), Staphylococcus epidermidis (MIC = 0.125 mg/mL), and Moraxella catarrhalis (MIC = 0.5 mg/mL) [27].
Additionally, another study showed that SH6 exhibited a significant inhibition level against S. aureus, E. coli, and C. perfringens [77]. Rubus ulmifolius fruit extract containing SH10, showed an antibacterial effect against Escherichia coli, Morganella morganii, and Proteus mirabilis, but higher extract concentrations were required: MIC = 5 mg/mL, MIC = 5 mg/mL, and MIC = 10 mg/mL, respectively [78].
5.4. Antifungal Activity
Moreover, Rubus ulmifolius fruit extract was tested as an antifungal agent. It was proved that the extract containing SH6 exhibited fungistatic activity against Candida albicans. The minimum inhibitory concentration was 5 mg/mL. Unfortunately, the extract did not show any fungicidal activity, achieving a result of >20 mg/mL [78].
5.5. Antiviral Activity (Including SARS-CoV-2)
Viruses, as pathogenic microorganisms, show significant genetic variability and the ability to mutate. Often, they do not show signs of infection at first. Currently, an increasing number of drug-resistant strains, as well as the toxicity of previously known drugs, force researchers to develop new antiviral substances [90]. In recent months, the entire world has been severely affected by the SARS-CoV-2 pandemic, which has led scientists to focus their attention on potential candidates against its eradication. More and more recent research conducted worldwide shows that sanguiins may be a potential candidate in the fight against viral diseases, including COVID-19 [91,92]. One of the studies predicted that SH6 is a compound that binds very well to the S1 and S2 subunits of the SARS-CoV-2 virus spine, which is responsible for entering the host cells and causing infection. SH6 showed the best binding energy among all tested compounds in the molecular docking assay. Additionally, SH2, also mentioned in the study, showed a lower result than the one mentioned above. Moreover, sanguiin has been proposed to act not only against the spike subunits of the SARS-CoV-2 virus [93]. Another molecular docking examination of polyphenolic compounds against the SARS-CoV-2 virus Mpro protease revealed that SH6 had the best result of all tested compounds in the in silico model [80]. Moreover, the study performed by S. Luo et al. concerned the verification of bacterial neuraminidase inhibitory properties by nine compounds isolated from mock strawberry (Duchesnea indica Andr.). SH4 exhibited significant inhibitory activity in an in vitro model, which offers potential for its use as a new antiviral substance [20].
5.6. Anticancer Activity
Additionally studied features of sanguiins are their potential anticancer activity. Several investigations on SH6 have explained its anticancer effect due to its promising competency in inhibiting DNA topoisomerases I and II. Moreover, the compound acted as a blocker to HeLa cells. It inhibited their growth at an effective dose of 12 µM and also had a dose-dependent effect on intracellular topoisomerase activity. SH6 also exhibited significant antiangiogenic potential [82]. A study by Lee S. et al. on HT1080 human fibrosarcoma cells showed that this compound blocked KDR/Flk-1-Fc binding to VEGF165 in a dose-dependent manner. Moreover, the compound obstructed the VEGF-induced proliferation of HUVEC cells (IC50 ca. = 7.4 µg/mL) but was not active against HT1080 human fibrosarcoma cells [83].
The potential antitumor properties of sanguiins were also tested on PRMI-7951 melanoma cells. A moderate selective cytotoxicity was shown by SH2, SH6, and SH11 with ED50 results of 0.44, 0.5, and 5.0 µg/mL, respectively [68]. Furthermore, anticancer activity was tested with SH4 isolated from Terminalia calamansanai leaves against large tumor cells lines, including human promyelocytic leukemia HL-60 cells. The compound induced a decrease in human poly (ADP-ribose) polymerase [79] (PARP) associated with the cleavage of procaspase-3 and exhibited strong activation of proapoptotic caspase-3 in HL-60 cells. It is worth mentioning that SH4 does not affect healthy cells, suggesting this compound is selective against cancer cells [24]. In another examination, SH6 was responsible for modulating the Smad 2/3 signaling pathway by TGF-β1, increasing the expression of the epithelial marker E-cadherin, repressing the expression of Snail and the mesenchymal marker N-cadherin during TGF-β1-induced EMT (epithelial-mesenchymal transition), and regulating the expression of EMT-dependent genes induced by TGF-β1. In summary, SH6 inhibits the migration and invasion of A549 lung cancer in vitro by inhibiting TGF-β1 induction of EMT [84].
Moreover, SH6 showed a large number of antiproliferative, antimigration, and cytotoxic effects against human breast carcinoma cells. A study performed by Berdowska et al. proved that the tested compound exhibited an inhibitory effect on adriamycin-resistant cells (MCF-7/Adr) [85]. It also showed antimetastatic properties in MDA-MB-231 cells by reducing the expression of vascular endothelial growth factor (VEGF), phosphorylated Akt, and kinase 1/2 (ERK1/2) regulated by extracellular signals [86]. In addition, SH6 increased the ratio of Bax to Bcl-2 in both MCF-7 and MDA-MB-231 cells [79].
SH6 was also studied for its activity against A2780 human ovarian carcinoma cells. The tested compound induced an antiproliferative effect and a morphological change similar to apoptotic cell death but did not arrest the cancer cell cycle. Moreover, SH6 showed an early apoptotic effect, caspase activation, PARP cleavage, activation of mitogen-activated protein kinases (MAPKs), especially p38, and an increase in truncated p15/BID [87].
5.7. Estrogenic Activity
SH6 has also been tested for estrogenic activity against MCF-7 human breast cancer cells. The E-screen examination and the molecular docking analysis showed that the SH6 from Rubus coreanus exhibited the best binding energy of −250,149 kcal/mol. Additionally, at 100 μg/mL, R. coreanus extract significantly stimulated cell proliferation (574.57% ± 8.56%). The study results indicated that SH6 contributed to the estrogenic activity of R. coreanus by activating the ERα coactivator binding site [81].
5.8. Neuroprotective Activity
Rubus L. subgenus R. watson, R. brigantinus, and R. vagabundus extracts containing SH2, SH6, and SH10 were tested for their potential neuroprotective properties against SK-N-MC neuroblastoma cells. All digested extracts after 2 and 24 h of preincubation reduced basal ROS production. Rubus brigantinus and R. vagabundus extracts increased the mitochondrial transmembrane potential and the integrity of the cell membrane. Moreover, the extracts increased GSH levels while not changing the GSH/GSSG ratio. It is worth mentioning that there is insufficient evidence for the interaction of brain endothelial cells with polyphenol metabolites, which makes it difficult to determine the level of the passage of the compound across the blood–brain barrier [62].
5.9. Clinical Trials
As mentioned above, the efficacy of sanguiins is mainly limited to preclinical studies. However, there has been some research on black raspberry and pomegranate food products in clinical trials. Considering the fact that these products are rich in ellagitannins, it can be concluded that the biological activity may also be connected with the occurrence of sanguiins in the juice from berries and pomegranate. Nevertheless, there is a lack of information on clinical studies that use only sanguiins in medical treatment [44,94,95].
6. Pharmacokinetics of Sanguiins
Sanguiins, belonging to the ellagitannin group, show similar pharmacokinetics. In vitro studies have shown that ellagitannins are stable in the gastric environment, and in the presence of gastric enzymes, they are not hydrolyzed to ellagic acid. In addition, the absorption of ellagitannins in the stomach is impracticable due to their complex chemical structure. However, free ellagic acid molecules can be absorbed in the stomach. On the other hand, the intestinal environment, together with the gastrointestinal microbiota, creates suitable conditions for their hydrolysis and decomposition into urolithins and their derivatives, which pass through the intestinal wall into the enterohepatic circulation [96]. In addition, in vivo studies have shown that the metabolism of SH6 and SH10 in the liver is partly based on conjugation with glucuronic acid and sulfuric acid, leading to the formation of compounds such as urolithin A-O-glucuronide, urolithin A-sulfate, and urolithin B-3-O-glucuronide. Moreover, urolithins were detected in the unconjugated form. Conjugation of derivatives occurs at different rates and intensities; Tmax of plasma urolithin glucuronides and sulfates is achieved in the vast majority of compounds 24 h after administration. Ultimately, conjugated and unconjugated compounds are excreted in the urine at varying intervals, up to 48 h after ingestion. Further in vivo clinical studies linked to full pharmacokinetic analysis are necessary to fully determine the participation of urolithins in the therapeutic effects of ellagitannin-rich plants [3,97,98].
7. Conclusions
The isolation and structure determination, accompanied by the measurement of the diverse pharmacological activities of each isolated sanguiin, has brought about a marked change in the concept of these compounds as active components of medicinal plants. In summary, sanguiins, especially sanguiin H-6, show evidence of promising action in various biological contexts, particularly in respect of their anticancer, antiradical, and antiviral properties. Apart from that, further studies involving drug delivery may improve the effectiveness of these compounds toward the drug target sites. Furthermore, it is worth considering performing a supplementary survey on their metabolism and toxicology patterns with molecular docking and molecular dynamics simulation to understand their mechanisms of action fully.
Author Contributions
Conceptualization, K.J., J.G. and M.T.; methodology, K.J. and J.G.; formal analysis, M.T. and A.G.A.; writing—original draft preparation, K.J. and J.G.; writing—review and editing, M.T. and A.G.A.; visualization, K.J., and J.G.; supervision, M.T. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Data are contained within the article.
Conflicts of Interest
The authors declare no conflict of interest.
Abbreviations
| SH2 | sanguiin H-2 |
| SH3 | sanguiin H-3 |
| SH5 | sanguiin H-5 |
| SH6 | sanguiin H-6 |
| SH10 | sanguiin H-10 |
| SH11 | sanguiin H-11 |
| ADMET | absorption, distribution, metabolism, excretion, toxicity |
| CINC-1 | cytokine-induced neutrophil chemoattractant |
| TNFα | tumor necrosis factor α |
| IL-1β | interleukin-1β |
| d.w. | dry weight |
| ONOO- | peroxynitrite |
| LPS | lipopolysaccharide |
| NFATc1 | nuclear factor of activated T cells 1 |
| NF-κB | nuclear factor-κB |
| c-Src | proto-oncogene tyrosine-protein kinase Src |
| TNF-α | tumor necrosis factor |
| PARP | poly (ADP-ribose) polymerase |
| EMT | epithelial-mesenchymal transition |
| TGF-β1 | transforming growth factor beta 1 |
| VEGF | vascular endothelial growth factor |
| iNOS | inducible NO synthase |
| ETs | ellagitannins |
| DPPH | 2,2-diphenyl-1-picrylhydrazyl |
| ROS | reactive oxygen species |
| ABTS | 2,29-azinobis-(3-ethylbenzo-thiazoline-6-sulfonic acid) |
| FRAP | ferric reducing ability of plasma |
| MRSA | methicillin-resistant Staphylococcus aureus |
| MSSA | methicillin-sensitive Staphylococcus aureus |
| MIC | minimum inhibitory concentration; |
| MBC | minimum bactericidal concentration |
| GSH | glutathione |
| GSSG | glutathione disulfide |
| BMMs | bone marrow macrophages |
| tBID | truncated BID |
| HUVECs | human umbilical vein endothelial cells |
| MCF-7/wt | MCF-7 human breast cancer cell (wild type) |
| FA | formic acid |
| TBA | thiobarbituric acid |
| ACN | acetonitrile |
| AMC | acceptable means of compliance |
| iNOS | inducible nitric oxide synthase |
| TRAP | tartrate-resistant acid phosphatase |
| ES/BS | eroded surface/bone surface |
| BMM | bone marrow-derived macrophages |
| NFATC1 Tmax | nuclear factor of activated T cells 1 time take to reach maximum concentration |
References
- Newman, D.J.; Cragg, G.M. Natural products as sources of new drugs over the 30 years from 1981 to 2010. J. Nat. Prod. 2012, 75, 311–335. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Atanasov, A.G.; Zotchev, S.B.; Dirsch, V.M.; Orhan, I.E.; Banach, M.; Rollinger, J.M.; Barreca, D.; Weckwerth, W.; Bauer, R.; Bayer, E.A.; et al. Natural products in drug discovery: Advances and opportunities. Nat. Rev. Drug Discov. 2021, 20, 200–216. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kiss, A.K.; Piwowarski, J.P. Ellagitannins, gallotannins and their metabolites—The contribution to the anti-inflammatory effect of food products and medicinal plants. Curr. Med. Chem. 2016, 25, 4946–4967. [Google Scholar] [CrossRef] [Scilit]
- Riaz, A.; Rasul, A.; Hussain, G.; Zahoor, M.K.; Jabeen, F.; Subhani, Z.; Younis, T.; Ali, M.; Sarfraz, I.; Selamoglu, Z. Astragalin: A bioactive phytochemical with potential therapeutic activities. Adv. Pharmacol. Sci. 2018, 2018, 9794625. [Google Scholar] [CrossRef] [Scilit]
- Clifford, M.N.; Scalbert, A. Ellagitannins—Nature, occurrence and dietary burden. J. Sci. Food Agric. 2000, 80, 1118–1125. [Google Scholar] [CrossRef]
- Prothmann, J.; Sun, M.; Spégel, P.; Sandahl, M.; Turner, C.; Scheuba, J.; Wronski, V.K.; Rollinger, J.M.; Grienke, U.; Santos-Buelga, C.; et al. Relationship between phenolic compounds, anthocyanins content and antioxidant activity in colored barley germplasm. J. Agric. Food Chem. 2017, 53, 1713. [Google Scholar]
- Su, X.; Surry, D.S.; Spandl, R.J.; Spring, D.R. Total synthesis of sanguiin H-5. Org. Lett. 2008, 10, 2593–2596. [Google Scholar] [CrossRef] [Scilit]
- Niemetz, R.; Gross, G.G. Enzymology of gallotannin and ellagitannin biosynthesis. Phytochemistry 2005, 66, 2001–2011. [Google Scholar] [CrossRef] [Scilit]
- Feldman, K.S.; Sambandam, A. Ellagitannin chemistry. the first total chemical synthesis of an O(2),O(3)-Galloyl-Coupled ellagitannin, sanguiin H-5. J. Org. Chem. 1995, 60, 8171–8178. [Google Scholar] [CrossRef] [Scilit]
- Bakkalbasi, E.; Mentes, O.; Artik, N. Food ellagitannins-occurrence, effects of processing and storage. Crit. Rev. Food Sci. Nutr. 2009, 49, 283–298. [Google Scholar] [CrossRef] [Scilit]
- Koponen, J.M.; Happonen, A.M.; Mattila, P.H.; Törrönen, A.R. Contents of anthocyanins and ellagitannins in selected foods consumed in Finland. J. Agric. Food Chem. 2007, 55, 1612–1619. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Su, X.; Surry, D.; Spandl, R.; Spring, D. Synthesis of Sanguiin H-5. Synfacts 2008, 2008, 1130. [Google Scholar] [CrossRef] [Scilit]
- Nonaka, G.; Tanaka, T.; Nita, M.; Nishioka, I. A dimeric hydrolyzable tannin, sanguiin H-6 from Sanguisorba officinalis L. Chem. Pharm. Bull. 1982, 30, 2255–2257. [Google Scholar] [CrossRef] [Scilit]
- Jakimiuk, K.; Wink, M.; Tomczyk, M. Flavonoids of the Caryophyllaceae. Phytochem. Rev. 2021, 20, 1–40. [Google Scholar] [CrossRef] [Scilit]
- Landete, J.M. Ellagitannins, ellagic acid and their derived metabolites: A review about source, metabolism, functions and health. Food Res. Int. 2011, 44, 1150–1160. [Google Scholar] [CrossRef] [Scilit]
- Patel, A.; Rojas-Vera, J.; Dacke, C.G. Therapeutic constituents and actions of Rubus species. Curr. Med. Chem. 2004, 11, 1501–1512. [Google Scholar] [CrossRef] [Scilit]
- Moreno-Medina, B.L.; Casierra-Posada, F.; Cutler, J. Phytochemical composition and potential use of Rubus species. Gesunde Pflanz. 2018, 70, 65–74. [Google Scholar] [CrossRef] [Scilit]
- Okuda, T.; Yoshida, T.; Hatano, T.; Iwasaki, M.; Kubo, M.; Orime, T.; Yoshizaki, M.; Naruhashi, N. Hydrolysable tannins as chemotaxonomic markers in the Rosaceae. Phytochemistry 1992, 31, 3091–3096. [Google Scholar] [CrossRef] [Scilit]
- Duckstein, S.M.; Lotter, E.M.; Meyer, U.; Lindequist, U. Phenolic constituents from Alchemilla vulgaris L. and Alchemilla mollis (Buser) Rothm. at different dates of harvest. Z. Naturforsch. C 2012, 67, 529–540. [Google Scholar] [CrossRef] [Scilit]
- Luo, S.; Guo, L.; Sheng, C.; Zhao, Y.; Chen, L.; Li, C.; Jiang, Z.; Tian, H. Rapid identification and isolation of neuraminidase inhibitors from mockstrawberry (Duchesnea indica Andr.) based on ligand fishing combined with HR-ESI-Q-TOF-MS. Acta Pharm. Sin. B 2020, 10, 1846–1855. [Google Scholar] [CrossRef] [Scilit]
- Lee, S.-H.; Tanaka, T.; Nonaka, G.; Nishioka, I.; Zhang, B. Allose gallates from Euphorbia fischeriana. Phytochemistry 1991, 30, 1251–1253. [Google Scholar] [CrossRef] [Scilit]
- Vrhovsek, U.; Guella, G.; Gasperotti, M.; Pojer, E.; Zancato, M.; Mattivi, F. Clarifying the identity of the main ellagitannin in the fruit of the strawberry, Fragaria vesca and Fragaria ananassa Duch. J. Agric. Food Chem. 2012, 60, 2507–2516. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mena, P.; Calani, L.; Dall’Asta, C.; Galaverna, G.; Garcia-Viguera, C.; Bruni, R.; Crozier, A.; Del Rio, D. Rapid and comprehensive evaluation of polyphenolic compounds in pomegranate (Punica granatum L.) juice by UHPLC-MS. Molecules 2012, 17, 14821–14840. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, L.G.; Huang, W.T.; Lee, L.T.; Wang, C.C. Ellagitannins from Terminalia calamansanai induced apoptosis in HL-60 cells. Toxicol. Vitr. 2009, 23, 603–609. [Google Scholar] [CrossRef] [Scilit]
- Tanaka, T.; Tachibana, H.; Nonaka, G.; Nishioka, I.; Hsu, F.-L.; Kohda, H.; Tanaka, O. Tannins and related compounds. CXXII. New dimeric, trimeric and tetrameric ellagitannins, lambertianins A-D, from Rubus lambertianus SERINGE. Chem. Pharm. Bull. 1993, 41, 1214–1220. [Google Scholar] [CrossRef] [Scilit]
- Verma, R.; Gangrade, T.; Punasiya, R.; Ghulaxe, X. Rubus fruticosus (blackberry) use as an herbal medicine. Pharmacogn. Rev. 2014, 8, 101–104. [Google Scholar] [CrossRef] [Scilit]
- Krauze-Baranowska, M.; Majdan, M.; Hałasa, R.; Głód, D.; Kula, M.; Fecka, I.; Orzeł, A. The antimicrobial activity of fruits from some cultivar varieties of Rubus idaeus and Rubus occidentalis. Food Funct. 2014, 5, 2536–2541. [Google Scholar] [CrossRef] [Scilit]
- Yoshida, T.; Amakura, Y.; Yoshimura, M. Structural features and biological properties of ellagitannins in some plant families of the order myrtales. Int. J. Mol. Sci. 2010, 11, 79–106. [Google Scholar] [CrossRef] [Scilit]
- Aires, A. (Ed.) Tannins: Structural Properties, Biological Properties and Current Knowledge, 1st ed.; IntechOpen: London, UK, 2020; pp. 21–53. [Google Scholar]
- Zhu, M.; Dong, X.; Guo, M.; Ferreira, I.; McPhee, D.J. Phenolic profiling of Duchesnea indica combining macroporous resin chromatography (MRC) with HPLC-ESI-MS/MS and ESI-IT-MS. Molecules 2015, 20, 22463–22475. [Google Scholar] [CrossRef] [Scilit]
- Liberal, J.; Francisco, V.; Costa, G.; Figueirinha, A.; Amaral, M.T.; Marques, C.; Girão, H.; Lopes, M.; Cruz, M.T.; Teresa, B.M. Bioactivity of Fragaria vesca leaves through inflammation, proteasome and autophagy modulation. J. Ethnopharmacol. 2014, 158, 113–122. [Google Scholar] [CrossRef] [Scilit]
- Yoshida, T.; Tanaka, K.; Chen, X.-M.; Okuda, T. Dimeric ellagitannins, laevigatins E, F and G, from Rosa laevigata. Phytochemistry 1989, 28, 2451–2454. [Google Scholar] [CrossRef] [Scilit]
- Cui, C.; Zhao, Q.-C.; Cai, B.; Yao, X.-S.; Osadsa, H. Two new and four known polyphenolics obtained as new cell-cycle inhibitors from Rubus aleaefolius poir. J. Asian Nat. Prod. Res. 2002, 4, 243–252. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, J.; Zhao, J.; Chen, W.; Lin, S.; Zhang, J.; Hong, Z. Hepatoprotection of 1β-hydroxyeuscaphic acid—The major constituent from Rubus aleaefolius against CCl4-induced injury in hepatocytes cells. Pharm. Biol. 2013, 51, 686–690. [Google Scholar] [CrossRef] [Scilit]
- Mertz, C.; Cheynier, V.; Günata, Z.; Brat, P. Analysis of phenolic compounds in two blackberry species (Rubus glaucus and Rubus adenotrichus) by high-performance liquid chromatography with diode array detection and electrospray ion trap mass spectrometry. J. Agric. Food Chem. 2007, 55, 8616–8624. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gancel, A.; Feneuil, A.; Acosta, O.; Mercedes, A.; Vaillant, F. Impact of industrial processing and storage on major polyphenols and the antioxidant capacity of tropical highland blackberry (Rubus adenotrichus). Food Res. Int. J. 2011, 44, 2243–2251. [Google Scholar] [CrossRef] [Scilit]
- Hukkanen, A.; Kostamo, K.; Karenlampi, S.; Kokko, H. Impact of agrochemicals on Peronospora sparsa and phenolic profiles in three Rubus arcticus cultivars. J. Agric. Food Chem. 2008, 56, 1008–1016. [Google Scholar] [CrossRef] [Scilit]
- Martins, A.; Barros, L.; Carvalho, A.M.; Santos-Buelga, C.; Fernandes, I.P.; Barreiro, F.; Ferreira, I.C.F.R. Phenolic extracts of Rubus ulmifolius Schott flowers: Characterization, microencapsulation and incorporation into yogurts as nutraceutical sources. Food Funct. 2014, 5, 1091–1100. [Google Scholar] [CrossRef] [Scilit]
- Puupponen-Pimiä, R.; Nohynek, L.; Suvanto, J.; Salminen Juha-Pekka Seppänen-Laakso, T.; Tähtiharju, J.; Honkapää, K.; Oksman-Caldentey, K.-M. Natural antimicrobials from cloudberry (Rubus chamaemorus) seeds by sanding and hydrothermal extraction. ACS Foods Sci. Technol. 2001, 1, 917–927. [Google Scholar] [CrossRef] [Scilit]
- Wang, B.; Koivumäki, T.; Kylli, P.; Heinonen, M.; Poutanen, M. Protein-phenolic interaction of tryptic digests of β-lactoglobulin and cloudberry ellagitannin. J. Agric. Food Chem. 2014, 62, 5028–5037. [Google Scholar] [CrossRef] [Scilit]
- Thiem, B. Rubus chamaemorus L.—A boreal plant rich in biologically active metabolites: A review. Biol. Lett. 2003, 40, 3–13. [Google Scholar]
- Grochowski, D.M.; Paduch, R.; Wiater, A.; Dudek, A.; Pleszczynska, M.; Tomczykowa, M.; Granica, S.; Polak, P.; Tomczyk, M. In vitro antiproliferative and antioxidant effects of extracts from Rubus caesius leaves and their quality evaluation. Evid. Based Complement. Altern. Med. 2016, 2016, 5698685. [Google Scholar] [CrossRef] [Scilit]
- Oszmiański, J.; Wojdyło, A.; Nowicka, P.; Teleszko, M.; Cebulak, T.; Wolanin, M. Determination of phenolic compounds and antioxidant activity in leaves from wild Rubus L. species. Molecules 2015, 20, 4951–4966. [Google Scholar] [CrossRef] [Scilit]
- Gu, J.; Ahn-Jarvis, J.H.; Riedl, K.M.; Schwartz, S.J.; Clinton, S.K.; Vodovotz, Y. Characterization of black raspberry functional food products for cancer prevention human clinical trials. J. Agric. Food Chem. 2014, 62, 3997–4006. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lim, T.K. Edible Medicinal and Non-Medicinal Plants: Fruits, 1st ed.; Springer: Dordrecht, The Netherlands, 2012; pp. 570–580. [Google Scholar]
- Krauze-Baranowska, M.; Głód, D.; Kula, M.; Majdan, M.; Hałasa, R.; Matkowski, A.; Kozłowska, W.; Kawiak, A. Chemical composition and biological activity of Rubus idaeus shoots—A traditional herbal remedy of Eastern Europe. BMC Complement. Altern. Med. 2014, 14, 1–12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sakai, E.; Aoki, Y.; Yoshimatsu, M.; Nishishita, K.; Iwatake, M.; Fukuma, Y.; Okamoto, K.; Tanaka, T.; Tsukuba, T. Sanguiin H-6, a constituent of Rubus parvifolius L., inhibits receptor activator of nuclear factor-κB ligand-induced osteoclastogenesis and bone resorption in vitro and prevents tumor necrosis factor-α-induced osteoclast formation in vivo. Phytomedicine 2016, 23, 828–837. [Google Scholar] [CrossRef] [Scilit]
- Jong-Won, C.; Yeong-Min, Y.; Min-Young, K.; Jung-Hwan, N.; Agung, N.; Hee-Juhn, P. Anti-hyperglycemic and anti-hyperlipidemic effects of the triterpenoid-rich fractions from Rubus coreanus and Rubus crataegifolius and their main component, niga-ichigoside f1, in streptozotocin-induced diabetic rats. Nat. Prod. Sci. 2008, 14, 260–264. [Google Scholar]
- Li, X.; Sun, J.; Chen, Z.; Jiang, J.; Jackson, A. Characterization of carotenoids and phenolics during fruit ripening of Chinese raspberry (Rubus chingii Hu). RSC Adv. 2021, 11, 10804–10813. [Google Scholar] [CrossRef] [Scilit]
- Jia-Yun, S.; Si-Qi, W.; Kao-Hua, L.; Bo, Z.; Qiao-Yan, Z.; Lu-Ping, Q.; Jian-Jun, W. Rubus chingii Hu: An overview of botany, traditional uses, phytochemistry, and pharmacology. Chin. J. Nat. Med. 2020, 18, 401–4016. [Google Scholar]
- Sun, Z.-L.; Zhang, Y.; Wan, A.-H.; Zhang, X.-L.; Feng, J. A new active compound against kidney deficiency from the fruits of Rubus corchorifolius. J. Asian Nat. Prod. Res. 2011, 13, 68–74. [Google Scholar] [CrossRef] [Scilit]
- Gasperotti, M.; Masuero, D.; Vrhovsek, U.; Guella, G.; Mattivi, F. Profiling and accurate quantification of Rubus ellagitannins and ellagic acid conjugates using direct UPLC-Q-TOF hdms and HPLC-DAD analysis. J. Agric. Food Chem. 2010, 58, 4602–4616. [Google Scholar] [CrossRef] [Scilit]
- Piwowarski, J.P.; Granica, S.; Zwierzyńska, M.; Stefańska, J.; Schopohl, P.; Melzig, M.F.; Kiss, A.K. Role of human gut microbiota metabolism in the anti-inflammatory effect of traditionally used ellagitannin-rich plant materials. J. Ethnopharmacol. 2014, 155, 801–809. [Google Scholar] [CrossRef] [Scilit]
- Zhang, G.; Liu, Y.; Hai, P. The complete chloroplast genome of tibetan medicinal plant Rubus phoenicolasius Maxim. Mitochondrial DNA Part B 2021, 6, 886–887. [Google Scholar] [CrossRef] [Scilit]
- Kool, M.M.; Comeskey, D.J.; Cooney, J.M.; McGhie, T.K. Structural identification of the main ellagitannins of a boysenberry (Rubus loganbaccus × baileyanus Britt.) extract by LC-ESI-MS/MS, MALDI-TOF-MS and NMR spectroscopy. Food Chem. 2010, 119, 1535–1543. [Google Scholar] [CrossRef] [Scilit]
- Lee, Y.A.; Lee, M.W. Tannins from Rubus coreanum. Korean J. Pharmacogn. 1995, 26, 27–30. [Google Scholar]
- Pang, K.C.; Kim, M.S.; Lee, M.W. Hydrolyzable tannins from the fruits of Rubus coreanum. Korean J. Pharmacogn. 1996, 27, 366–370. [Google Scholar]
- Kim, M.S.; Pang, K.C.; Lee, S.M. Tannins from the leaves of Rubus coreanum. Korea Sci. 1996, 40, 666–669. [Google Scholar]
- Kim, L.S.; Youn, S.H.; Kim, J.Y. Comparative study on antioxidant effects of extracts from Rubus coreanus and Rubus occidentalis Lee. J. Korean Soc. Food Sci. Nutr. 2014, 43, 1357–1362. [Google Scholar] [CrossRef] [Scilit]
- Kosmala, M.; Jurgoński, A.; Juśkiewicz, J.; Karlińska, E.; Macierzuński, J.; Rój, E.; Zduńczyk, Z. Chemical composition of blackberry press cake, polyphenolic extract, and defatted seeds, and their effects on cecal fermentation, bacterial metabolites, and blood lipid profile in rats. J. Agric. Food Chem. 2017, 65, 5470–5479. [Google Scholar] [CrossRef] [Scilit]
- Sparzak, B.; Merino-Arevalo, M.; Vander Heyden, Y.; Krauze-Baranowska, M.; Majdan, M.; Fecka, I.; Głód, D.; Ba̧czek, T. HPLC analysis of polyphenols in the fruits of Rubus idaeus L. (Rosaceae). Nat. Prod. Res. 2010, 24, 1811–1822. [Google Scholar] [CrossRef] [Scilit]
- Tavares, L.; Figueira, I.; McDougall, G.; Vieira, H.; Stewart, D.; Alves, P.; Ferreira, R.; Santos, C. Neuroprotective effects of digested polyphenols from wild blackberry species. Eur. J. Nutr. 2013, 52, 225–236. [Google Scholar] [CrossRef] [Scilit]
- Nonaka, G.I.; Tanaka, T.; Nishioka, I. Tannins and related compounds. Part 3. A new phenolic acid, sanguisorbic acid dilactone, and three new ellagitannins, sanguiins H-1, H-2, and H-3, from Sanguisorba officinalis. J. Chem. Soc. Perkin Trans. 1 1982, 1067–1073. [Google Scholar] [CrossRef] [Scilit]
- Zhao, Z.; He, X.; Zhang, Q.; Wei, X.; Huang, L.; Fang, J.; Wang, X.; Zhao, M.; Bai, Y.; Zheng, X. Traditional uses, chemical constituents and biological activities of plants from the genus Sanguisorba L. Am. J. Chin. Med. 2017, 45, 199–224. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Arun, N.; Road, R.; Pradesh, U. Punica granatum: A review on pharmacological and therapeutic properties. Int. J. Pharm. Sci. Res. 2012, 3, 1240–1245. [Google Scholar]
- Lia, Y.-N.; He, J.; Zhang, J.; Shi, Y.-X.; Guo, L.-B.; Peng, Z.-C.; Yang, T.; Ding, K.; Zhang, W.-K.; Xu, J.-K. Existing knowledge on Euphorbia fischeriana Steud. (Euphorbiaceae): Traditional uses, clinical applications, phytochemistry, pharmacology and toxicology. J. Ethnopharmacol. 2021, 275, 114095. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Juszczak, A.M.; Zovko-Končić, M.; Tomczyk, M. Recent trends in the application of chromatographic techniques in the analysis of luteolin and its derivatives. Biomolecules 2019, 9, 731. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kashiwada, Y.; Nonaka, G.I.; Nishioka, I.; Chang, J.J.; Lee, K.H. Tannins and related compounds as selective cytotoxic agents. J. Nat. Prod. 1992, 55, 1033–1043. [Google Scholar] [CrossRef] [Scilit]
- Jang, E.; Inn, K.S.; Jang, Y.P.; Lee, K.T.; Lee, J.H. Phytotherapeutic activities of Sanguisorba officinalis and its chemical constituents: A review. Am. J. Chin. Med. 2018, 46, 299–318. [Google Scholar] [CrossRef] [Scilit]
- Konishi, K.; Urada, M.; Adachi, I.; Tanaka, T. Inhibitory effect of sanguiin H-11 on chemotaxis of neutrophil. Biol. Pharm. Bull. 2000, 23, 213–218. [Google Scholar] [CrossRef] [Scilit]
- Sangiovanni, E.; Vrhovsek, U.; Rossoni, G.; Colombo, E.; Brunelli, C.; Brembati, L.; Trivulzio, S.; Gasperotti, M.; Mattivi, F.; Bosisio, E.; et al. Ellagitannins from Rubus berries for the control of gastric inflammation: In vitro and in vivo studies. PLoS ONE 2013, 8, e71762. [Google Scholar] [CrossRef] [Scilit]
- Yokozawa, T.; Chen, C.P.; Rhyu, D.Y.; Tanaka, T.; Park, J.C.; Kitani, K. Potential of sanguiin H-6 against oxidative damage in renal mitochondria and apoptosis mediated by peroxynitrite in vivo. Nephron 2002, 92, 133–141. [Google Scholar] [CrossRef] [Scilit]
- Mullen, W.; McGinn, J.; Lean, M.E.J.; MacLean, M.R.; Gardner, P.; Duthie, G.G.; Yokota, T.; Crozier, A. Ellagitannins, flavonoids, and other phenolics in red raspberries and their contribution to antioxidant capacity and vasorelaxation properties. J. Agric. Food Chem. 2002, 50, 5191–5196. [Google Scholar] [CrossRef] [Scilit]
- Song, J.H.; Kim, S.Y.; Hwang, G.S.; Kim, Y.S.; Kim, H.Y.; Kang, K.S. Sanguiin H-11 from Sanguisorbae radix protects HT22 murine hippocampal cells against glutamate-induced death. Bioorgan. Med. Chem. Lett. 2019, 29, 252–256. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kähkönen, M.; Kylli, P.; Ollilainen, V.; Salminen, J.P.; Heinonen, M. Antioxidant activity of isolated ellagitannins from red raspberries and cloudberries. J. Agric. Food Chem. 2012, 60, 1167–1174. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yokozawa, T.; Chen, C.P.; Tanaka, T.; Kitani, K. Effects of sanguiin H-6, a component of Sanguisorbae radix, on lipopolysaccharide-stimulated nitric oxide production. Biochem. Pharmacol. 2002, 63, 853–858. [Google Scholar] [CrossRef] [Scilit]
- Puljula, E.; Walton, G.; Woodward, M.J.; Karonen, M. Antimicrobial activities of ellagitannins against Clostridiales perfringens, Escherichia coli, Lactobacillus plantarum and Staphylococcus aureus. Molecules 2020, 25, 3714. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Da Silva, L.P.; Pereira, E.; Pires, T.C.S.P.; Alves, M.J.; Pereira, O.R.; Barros, L.; Ferreira, I.C.F.R. Rubus ulmifolius Schott fruits: A detailed study of its nutritional, chemical and bioactive properties. Food Res. Int. 2019, 119, 34–43. [Google Scholar] [CrossRef] [Scilit]
- Park, E.J.; Lee, D.; Baek, S.E.; Kim, K.H.; Kang, K.S.; Jang, T.S.; Lee, H.L.; Song, J.H.; Yoo, J.E. Cytotoxic effect of sanguiin H-6 on MCF-7 and MDA-MB-231 human breast carcinoma cells. Bioorgan. Med. Chem. Lett. 2017, 27, 4389–4392. [Google Scholar] [CrossRef] [Scilit]
- Bhatia, S.; Giri, S.; Singh, S.; Lal, A.F. Identification of potential inhibitors of dietary polyphenols for SARS-CoV-2 M protease: An in silico study. One Health Bull. 2020, 1, 21–29. [Google Scholar]
- Trinh, T.A.; Park, E.-J.; Lee, D.; Song, J.H.; Lee, H.L.; Kim, K.H.; Kim, Y.; Jung, K.; Kang, K.S.; Yoo, J.-E. Estrogenic activity of sanguiin H-6 through activation of estrogen receptor α coactivator-binding site. Nat. Prod. Sci. 2019, 25, 28. [Google Scholar] [CrossRef] [Scilit]
- Bastow, K.F.; Bori, I.D.; Fukushima, Y.; Kashiwada, Y.; Tanaka, T.; Nonaka, G.; Nishioka, I.; Lee, K.H. Inhibition of DNA topoisomerases by sanguiin H-6, a cytotoxic dimeric ellagitannin from Sanguisorba officinalis. Planta Med. 1993, 59, 240–245. [Google Scholar] [CrossRef] [Scilit]
- Lee, S.J.; Lee, H.K. Sanguiin H-6 blocks endothelial cell growth through inhibition of VEGF binding to VEGF receptor. Arch. Pharm. Res. 2005, 28, 1270–1274. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ko, H.; Jeon, H.; Lee, D.; Choi, H.K.; Kang, K.S.; Choi, K.C. Sanguiin H6 suppresses TGF-β induction of the epithelial-mesenchymal transition and inhibits migration and invasion in A549 lung cancer. Bioorgan. Med. Chem. Lett. 2015, 25, 5508–5513. [Google Scholar] [CrossRef] [Scilit]
- Berdowska, I.; Zieliński, B.; Saczko, J.; Sopel, M.; Gamian, A.; Fecka, I. Modulatory impact of selected ellagitannins on the viability of human breast cancer cells. J. Funct. Foods 2018, 42, 122–128. [Google Scholar] [CrossRef] [Scilit]
- Park, E.-H.H.; Park, J.Y.; Yoo, H.-S.S.; Yoo, J.-E.E.; Lee, H.L. Assessment of the anti-metastatic properties of sanguiin H-6 in HUVECs and MDA-MB-231 human breast cancer cells. Bioorgan. Med. Chem. Lett. 2016, 26, 3291–3294. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lee, D.; Ko, H.; Kim, Y.-J.; Kim, S.-N.; Choi, K.-C.; Yamabe, N.; Kim, K.H.; Kang, K.S.; Kim, H.Y.; Shibamoto, T. Inhibition of A2780 human ovarian carcinoma cell proliferation by a Rubus component, sanguiin H-6. J. Agric. Food Chem. 2016, 64, 801–880. [Google Scholar] [CrossRef] [Scilit]
- Yokozawa, T.; Chen, C.P.; Tanaka, T. Direct scavenging of nitric oxide by traditional crude drugs. Phytomedicine 2000, 6, 453–463. [Google Scholar] [CrossRef] [Scilit]
- Frieri, M.; Kumar, K.; Boutin, A. Antibiotic resistance. J. Infect. Public Health 2017, 10, 369–378. [Google Scholar] [CrossRef] [Scilit]
- Oh, D.Y.; Hurt, A.C. A review of the antiviral susceptibility of human and avian influenza viruses over the last decade. Scientifica 2014, 2014, 430629. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tu, Y.-F.; Chien, C.-S.; Yarmishyn, A.A.; Lin, Y.-Y.; Luo, Y.-H.; Lin, Y.-T.; Lai, W.-Y.; Yang, D.-M.; Chou, S.-J.; Yang, Y.-P.; et al. A review of SARS-CoV-2 and the ongoing clinical trials. Int. J. Mol. Sci. 2020, 21, 2657. [Google Scholar] [CrossRef] [Scilit]
- Lim, Y.X.; Ng, Y.L.; Tam, J.P.; Liu, D.X. Human coronaviruses a review of virus-host interactions. Diseases 2016, 4, 26. [Google Scholar] [CrossRef] [Scilit]
- Arnica, F.; Sabeena, G.; Sonam, B.; Shaminder, S.; Sonia, M. Identification of ellagitannins as natural inhibitors of spike proteins of COVID19 virus: An in silico- based study for drug development. Afr. J. Health Sci. 2020, 33, 78–97. [Google Scholar]
- Stoner, G.D.; Sardo, C.; Apseloff, G.; Mullet, D.; Wargo, W.; Pound, V.; Singh, A.; Sanders, J.; Aziz, R.; Casto, B.; et al. Pharmacokinetics of anthocyanins and ellagic acid in healthy volunteers fed freeze-dried black raspberries daily for 7 days. J. Clin. Pharmacol. 2005, 45, 1153–1164. [Google Scholar] [CrossRef] [Scilit]
- Cho, J.M.; Chae, J.; Jeong, S.R.; Moon, M.J.; Ha, K.C.; Kim, S.; Lee, J.H. The cholesterol-lowering effect of unripe Rubus coreanus is associated with decreased oxidized LDL and apolipoprotein B levels in subjects with borderline-high cholesterol levels: A randomized controlled trial. Lipids Health Dis. 2020, 19, 1–12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lipińska, L.; Klewicka, E.; Sójka, M. The structure, occurrence and biological activity of ellagitannins: A general review. Acta Sci. Pol. Technol. Aliment. 2014, 13, 289–299. [Google Scholar] [CrossRef] [Scilit]
- Espín, J.C.; Larrosa, M.; García-Conesa, M.T.; Tomás-Barberán, F. Biological significance of urolithins, the gut microbial ellagic acid-derived metabolites: The evidence so far. Evid.-Based Complement. Altern. Med. 2013, 2013, 270418. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ludwig, I.A.; Mena, P.; Calani, L.; Borges, G.; Pereira-Caro, G.; Bresciani, L.; Del Rio, D.; Lean, M.E.J.; Crozier, A. New insights into the bioavailability of red raspberry anthocyanins and ellagitannins. Free Radic. Biol. Med. 2015, 89, 758–769. [Google Scholar] [CrossRef] [Scilit]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2021 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).