


Abstract
Vector control methods are considered effective in averting dengue transmission. However, several factors may modify their impact. Of these controls, chemical methods, in the long run, may increase mosquitoes’ resistance to chemicides, thereby decreasing control efficacy. The biological methods, which may be self-sustaining and very effective, could be hampered by seasonality or heatwaves (resulting in, e.g., loss of Wolbachia infection). The environmental methods that could be more effective than the chemical methods are under-investigated. In this study, a systematic review is conducted to explore the present understanding of the effectiveness of vector control approaches via dengue transmission models.
1. Introduction
Dengue is one of the world’s most threatening and widespread mosquito-borne diseases [1,2]. In recent decades, dengue has accounted for approximately 390 million new infections each year, with 96 million of these being symptomatic [3,4]. Most of the new annual infected cases (approximately 70% of 390 million) are distributed across Asia, while Africa, the Americas, and Oceania shared infection distributions of approximately 16.4%, 13.8%, and 0.2%, respectively [3]. The main vectors responsible for dengue transmission are Aedes aegypti and Aedes albopictus [5]. Dengue virus (DENV) has four distinct but closely related serotypes of the genus Flavivirus, namely: DENV-1; DENV-2; DENV-3; and DENV-4. When one recovers from one of these serotypes, it may provide lifelong immunity against that serotype. However, the cross-reactive immunity of the other serotypes is only temporary and partial [6]. Therefore, the subsequent infection of different serotypes of the dengue virus poses an increase in the risk of severe dengue viral infection [6]. The clinical manifestation includes headache, arthralgia, sudden high-grade fever, eye pain, nausea, and muscle ache [7]. Currently, there is no specific treatment for dengue. The efficacy of the vaccine that targets young patients depends on prior immunity to dengue, and it provides heterogeneous protection against the different serotypes [8,9]. The extent and severity of the burden imposed by dengue infection and disease have renewed calls for immediate intervention and control [10,11,12,13].
Vector control remains the most widely adopted technique to suppress the transmission of dengue [4,14]. This is because reducing the prevalence of dengue-carrying mosquitoes or inhibiting their transmission capacities typically poses a negligible risk of environmental contamination and demands little provision to sustain control [4,15].
There are three main approaches to vector control, namely, the chemical, environmental, and biological approaches [4,16]. Chemical methods involve the direct killing of mosquito vectors either by insecticide via indoor-residual spraying (IRS) or by limiting the reproduction of the vector population by chemically destroying mosquito breeding sites [4,17,18]. Environmental methods include emptying or covering water-filled containers, installing adequate water supply pipes, implementing efficient waste management strategies, and ensuring a clean environment [4]. Biological methods rely on the introduction of biological control agents, such as lavivorous fish, copepods, genetically modified mosquitoes, and Wolbachia-infected mosquitoes, which are incapable of transmitting arboviral pathogens [19,20,21]. Of these biological control methods, the Wolbachia-based strategy is becoming increasingly popular for controlling viral diseases (such as dengue) because it is potentially self-sustaining [15,22,23,24]. Although there is an emerging control method, mechanical control, that involves the mass trapping of mosquitoes using lethal traps and has been successful in controlling vectors transmitting dengue [25,26,27], mathematical models describing this method are scarce [28].
In practice, vector control—which addresses the suppression of the vector population and disruption of the viral transmission capabilities of mosquitoes—is the primary method for reducing dengue viral transmission. Unfortunately, these methods typically require considerable labour and monetary investments to achieve successful and sustained control and may also pose environmental risks (e.g., through the use of chemicides) [4,16]. The authors in [29] reviewed published articles on arboviral infections (such as dengue, Zika, and chikungunya) and their vector (Aedes mosquitoes) controls in general. They further assessed Wolbachia-based control studies for mitigating or eliminating arboviral infections and discussed gaps, such as the combination of the three (biological, chemical, and environmental) vector control methods and the use of two different Wolbachia strains that could be instrumental in developing models to estimate the impact of the controls. In this study, we examine the role of mathematical models in controlling the transmission of dengue and explore the present understanding of the effectiveness of vector controls in the last decade. This requires an extensive systematic search of the literature using field-related search terms in three different databases.
The introduction of mathematical models to understand viral infection dynamics has long been helpful in the area of disease control [30,31,32,33,34,35,36]. Several models involving vector control of the transmission of different dengue serotypes have been formulated and analysed [30,32,33,34,35,36,37,38,39,40,41,42,43,44,45,46,47,48,49,50,51,52,53,54,55,56,57,58,59,60,61,62,63,64,65]. Some studies [35,36,38,41,42,44,52] investigated dengue transmission models capturing the different dengue serotypes together with their vectors. Further, they described the dengue models by either host-vector transmission dynamics or purely by interactions between vectors. Here we review mathematical models of dengue vector control and identify literature modelling gaps in the last decade (from 2010 to 2020). We limited the time range to the last decade because some vector control techniques, such as Wolbachia-based techniques, were only recently successfully introduced [24,66], and a systematic review of dengue transmission models which accounts for vector control has been described up to early 2012 [36]. Another similar study by Perkins et al. [67] reviewed the dengue transmission models that covered a 40-year period (i.e., from 1970–2010). They used a standardized questionnaire to describe the various biological assumptions (corresponding to the Ross-Macdonald model assumptions) guiding each model and then gave both qualitative and quantitative findings. We carefully appraise published research articles describing the dengue transmission models and specifically classify these models according to the vector control method studied within a decade (i.e., from 2010–2020). This, in turn, will help reveal the literature gaps that will inform the development and modification of dengue models to account for effective vector control techniques.
2. Methods
The Preferred Reporting Items for Systematic Reviews and Meta-Analyses (PRISMA) guidelines [68] were used to conduct a systematic literature search. This search was performed using the MEDLINE, Web of Science (WOS), and SCOPUS databases from March to December 2020. We systematically used various keywords and/or synonyms, such as “dengue” OR “arbovirus”, together with “model” AND “control” OR “strategy” OR “technique” (see Additional File S1). Other keywords, such as “flavivirus”, “dengue virus”, “insect control”, and “communicable disease control”, were used to expand the search terms as some of the terms have been used interchangeably in the pool of literature. This review is aimed at the mathematical modelling of vector control methods in dengue transmission models. For each vector control method, we identify the underlying structure of the mathematical model, parameter assumptions, thresholds of implementations, and limitations.
2.1. Selection Criteria
At the initial stage of the search process, there were no restrictions for the time frame of the selected articles from each database used. However, it was later limited to 2010–2020. This is because (i) biological vector control techniques, in particular, Wolbachia-based control, were not significantly discussed until the last decade when the successful establishment of Wolbachia infection and its ability to block viral transmission in Aedes mosquitoes were reported [24,66], and (ii) another systematic review of the structure of dengue epidemiological transmission models, which includes vector control strategies, was conducted up to March 2012 [36].
The titles and abstracts of the articles irrelevant to the scope of the study were excluded from the articles of discussion (see details in the Section 3). Study articles published in non-English languages were removed from the considered pool of articles. Other referencing types, such as conference proceedings, serials, books, and book sections, were also removed. The inclusion criteria for these articles include the following:
- A representation of vectors or vector-host dynamics to control dengue transmission.
- A deterministic (DM), stochastic (SM), or network (NM) modelling approach using systems of ODEs.
- A vector control strategy leading to dengue viral reduction or elimination.
2.2. Data Extraction
The selected articles for this study were evaluated according to the modelling characteristics in terms of contributions made. These studies’ features include the aim and objectives, modelling methods, study location, vector control types, and key findings. It is important to mention that the vector control effectiveness of these studies was extracted from the findings and conclusions (Table 1). This is because the conclusive findings described in the studies provide a means for comparison and inference based on study effectiveness. Models were also categorised based on the year, vector control types, methods, and location of study to capture the general trend and geographical clusters of these models (Table 1). Figure 1 shows the distribution of the selected articles, stratified using the vector control types and location in which the controls were conducted. In other words, this shows the geographic clustering for where the experimental data were obtained for validating the vector control model outputs (Figure 1).
Table 1.
Characteristics of selected articles describing the year, aims and objectives, modelling methods, settings location, main vector control method and summary of studies. DM → deterministic model, SM → stochastic model, and NM → network model. C → chemical control, B → biological control, and E → environmental control. n/a→not available.
Figure 1.
The distribution of the locations of the selected experimental studies used for validating models describing the vector control types.
2.3. Assessment of Study Quality
We adapted and built upon the tool for the Assessment of Modelling Studies (AMS) [69], which is used for assessing modelling work in health and economics. In particular, we built upon the AMS by adding two more criteria (modelling methods and reporting conflicts of interest) to the ten existing criteria in the AMS (Table 2). The newly modified ASM tool used the quality assessment value formats in [70]. The tool comprises 12 criteria, and these criteria describe the characteristics of each of the articles selected for this review. Each criterion in the adapted tool used was assigned a rating from 0 to 2, where the following values represent the AMS criteria: 0 → absent, 1→ partially present, and 2 → fully present. Herein, the highest score for the modelling studies is 24 points. To compute the score (in percentage) for an article, we used where is the number of points estimated for an article. Below, the quality of the articles is stratified into four categories: low ( 50%), medium (50% < y 65%), high (65% < y 80%), and very high (y > 80%) (Table 2).
Table 2.
Description of the quality assessment of the included studies adopting the tool Assessment for Modelling Studies (ASM). The values in the table below represent the AMS criteria 0 → absent, 1 → partially present, 2 → fully present.
3. Results
3.1. Search Strategies and General Study Characteristics
A total of 2158 articles were identified from the standard databases: MEDLINE—1069, WOS—643, and SCOPUS—446. Of these, 336 duplicated studies were found and subsequently removed. Of the remaining 1822 studies screened, 644 records were excluded. This exclusion includes 8 books, 27 book sections, 19 conference proceedings, 4 serials, 134 non-English articles, and 452 articles whose years were after 2010. The 1178 remaining articles were screened by reading the titles and abstracts. Of these, 1106 studies were excluded because they were deemed irrelevant, i.e., not containing information governing the inclusion criteria and the scope of the review. In total, 72 full-text study assessments were performed. Of these, we excluded 40 articles that either did not describe deterministic, stochastic, network models, or the vector control methods as a technique for dengue control and whose aim is closely related to the selected articles. Finally, 32 articles were selected and considered in this review (Figure 2). The distribution of these review articles by calendar year is shown in Figure 3. In Figure 3, more than half of the 32 selected modelling articles were published in or after 2017, i.e., over the past four years.
Figure 2.
PRISMA flowchart for article selection process.
Figure 3.
The yearly distribution of the number of selected published modelling articles with respect to the vector control types.
3.2. Distribution of Vector Control Modelling Articles
In this review, 32 modelling articles were considered and included in the study. These articles were published between 2010 and 2020 (Figure 3). The stacked bar chart in Figure 3 shows the distribution of the three different vector control strategies over the years. Beginning with the biological vector control, there is an increasing trend in the number of published articles, and this is mostly seen in the last two years. This increase may have been fuelled by the largest dengue viral outbreak in the Americas, southeast Asia, Europe, sub-Saharan Africa, and Oceania regions and by greater recognition of this novel strategy [71]. The number of publications addressing chemical methods of vector control remains approximately constant over the years, reflecting its ongoing dominant role in contemporary vector control [72]. Only three papers address environmental controls (Figure 3), and two of the three are from the last two years of publications in this study, suggesting this may be a growing area of interest [4]. Most (28 out of 32) of the overall articles selected are deterministic modelling studies of dengue transmission [32,34,35,37,38,39,40,41,42,43,44,46,48,49,50,51,52,53,54,56,57,58,59,61,62,63,64,65]. Three of the thirty-two articles are stochastic modelling studies [33,47,60]. Only one is a network modelling study [55].
Ten (10) of the 32 articles investigated the chemical method for vector control [33,37,46,47,48,49,54,56,61,62,63]; nineteen (19) articles described the biological method of control [32,34,35,38,40,41,42,43,44,50,51,52,53,55,57,58,64,65]; while only three (3) of the articles partially discussed the environmental method for vector control [39,59,60]. More than half (60%) of the selected modelling studies were categorised under biological control methods. The chemical methods of control articles were 31%, while the least (9%) was that of the environmental methods. We now discuss the vector control methods elaborately below.
4. Vector Control Methods
The selected dengue modelling studies have been characterised by the aims and objectives, year of publication, modelling methods, study location, vector control types, and summary of the articles to gain clarity (Table 1).
4.1. Chemical Control Methods
This method describes the use of a chemical solution, mixture, aerosol, or material to directly repel, expel, or, in some cases, kill arthropod vectors, such as mosquitoes [73,74,75]. Chemical control includes the use of pyrethroids for outdoor fogging [76,77], insecticides for indoor and outdoor residual spraying [17,78], insecticide-treated bed nets (ITN) [79,80], insecticide-treated house screens (ITHS) [81], and insecticide-treated door curtains (ITC) [82], and chemical larvicides, such as temephos, to directly kill or destroy mosquito vectors and their breeding sites [83,84].
Ten dengue transmission modelling studies in the selected articles incorporate chemical control methods [33,37,46,47,48,49,54,56,61,63]. Of these, eight were based on deterministic models (DM) [37,46,48,49,54,56,61,63], while the other two used stochastic modelling (SM) [33,47]. Some studies based on the DM featured vector populations only [63] or both human and vector populations [37,46,48,49,54,56,61], while SM studies considered coevolution dynamics of both humans and mosquitoes. For some of the DMs modelling both human and vector populations, the basic reproductive number (R0) with respect to dengue was computed and further illustrated that the disease-free equilibrium (DFE) is stable if it is less than unity (i.e., R0 < 1) [46,49,54,61] or in the presence of backward bifurcation where DFE may coexist with an endemic equilibrium [37]. A study estimated the value of R0 during the 2014 Guangdong Province dengue outbreak in China to be around 1.74, and after implementing impulsive vector control strategies, it reduced to 0.17 [61], while the R0 for the 2017 dengue outbreak in Pakistan was estimated to be approximately 2.65 [37] and another study estimated the R0 to be 8.16 [49]. One modelling study, alongside experimental data from Brazil, predicted that the dissemination of pyriproxyfen would, under some optimistic, realistic, and worse-case epidemiological scenarios (based on parameter modification, such as daily vector death rate, vector-to-human ratio, among others), reduce the values of R0 with respect to Aedes-borne viruses, such as dengue, Zika, and chikungunya (which was estimated to be between 3–45, i.e., range of optimistic to worse-case scenarios) by 100–1000 fold [46].
Almost half (13 out of 32) of the selected studies performed sensitivity analysis [33,35,37,38,42,43,44,53,54,57,59,61,65]. Four of the studies [35,37,59,61] used the Latin hypercube sampling (LHS) and partial rank correlation coefficients (PRCC) and provided evidence that the most effective parameters in curtailing dengue viral spread include reducing the transmission probability per contact of either infectious mosquitoes with susceptible humans or susceptible mosquitoes with infectious humans; mosquito recruitment and death rates; and human recovery rates [37,61]. Other highly sensitive parameters include the epidemic size, date of arrival of the infectious human and mean annual temperature [59]. One study used probabilistic sensitivity and threshold analyses and showed that if the cost of adult mosquito control was greater than 16 times that of larval control, all the adult vector control strategies were dominated [54]. Another study investigated the sensitivity of the vector model with respect to the parameter values used for the SIT method for dengue vector control and showed that shorter mosquito lifespans significantly prevent the disease from occurring; however, the disease could possibly persist (few cases) if the mosquito lifespan is less than its extrinsic incubation period [38].
To account for the robustness of the transmission models with respect to the corresponding biological implications, two studies [44,65] performed sensitivity analyses on a large range of parameter values and found that fitness cost and maternal transmission parameters are the main factors that determine the establishment of Wolbachia-infected mosquitoes in a wild-type population [44,65]. The effect of these factors could induce a backward bifurcation when the fitness cost is high [65]. A study by Li et al. investigated the robustness of the release strategy of the model for different values of CI. The authors showed that there was no significant difference between the different values of CI chosen and, as such, suggested excellent robustness [53]. Similarly, some researchers explored the uncertainty in asymptomatic cases of dengue viral transmission in Brazil. They simulated two scenarios with 50% and 100% transmission rates for asymptomatic individuals and found that there was a similar reduction in dengue cases for both rates [33]. A study that described the dengue transmission dynamics using boosted SIT approaches performed a sensitivity analysis on the model parameters and showed that for low release rates boosting the SIT methods reduced the elimination threshold the most [57]. Some of the modelling studies [46,47,48,61,63] revealed that the use of insecticides or fumigation significantly reduced the emergence and production of vectors (in particular, Aedes aegypti mosquitoes) and, in turn, reduced the burden of dengue [33,46,49,56]. However, continual long-term mosquito larvae control may prove ineffective due to the evolution of mosquito resistance [54].
Further, some modelling studies considered cost-effectiveness and benefits as part of their analysis [37,38,41,43,48,54,62,63]. Cost-effectiveness analysis—which includes the calculation of the infection averted ratio (IAR), average cost-effectiveness ratio (ACER), and incremental cost-effectiveness ratio (ICER)—describes the advantages and costs with respect to the control strategies, allowing one to identify the most effective strategy [37,38,48,54]. The authors in [48] investigated the cost–benefits of dengue control strategies via insecticide-treated bed-nets (ITN) and spraying interventions. They found that the combination of both strategies with low-cost weight was most effective in reducing dengue infections (IAR = 0.76, ACER = 5.65); however, the insecticide spraying strategy only was the most cost-effective (IAR = 0.71, ACER = 4.35) [48]. Another study investigated the potential costs per dengue case averted by the SIT control strategy based on the average cost estimates derived from SIT data. They showed that the yearly mean per capita cost of the vector control measures was USD 0.765. That is, the yearly control cost of the simulated two million people would be USD 1.53 million, and for about 5000 people, that would be USD 3825. This would save a large percentage of infection [38]. A study described 43 insecticide-based interventions together with the cost-effectiveness of different (larval and adult mosquito) control strategies and stratified the control efficacy into high (90% mosquito mortality [MM]), intermediate (60% MM), and low (30% MM) with annual application frequencies [54]. They showed that the high-efficacy adult vector control strategies dominated the larval control strategies because of the increasing resistance of larvae within the 5-year time horizon. Of the frequencies examined, twice annual control was the most efficient (ICER = USD 615), whereas six times annual control was the most effective (ICER = USD 1267), with the increased cost per disability-adjusted life years (DALY) saved meeting the willingness to pay threshold. This suggests that of all the vector controls, the one that most significantly reduced the DALYs lost was the high-efficacy adult mosquito control with six application frequencies [54]. The authors in [43] investigated the impact of the Wolbachia-based strategy in reducing the dengue burden and estimated over 330 thousand DALYs lost attributable to dengue in Indonesia. Of the DALYs lost, approximately a quarter is caused by a fatality, while the rest is due to disability [43].
A number of studies explored the optimal control strategies associated with the cost benefits of dengue control strategies [37,41,62,63]. A study of dengue where model outputs were validated with experimental data in Pakistan introduced two time-dependent control variables: the use of insecticide and vaccination [37]. They investigated the effect of costs on the cost weights of insecticide and vaccination use and found that as the cost of insecticides increases, the use of vaccination also increases. However, when vaccination decreased as a result of an increase in cost, an exiguous increase in the use of insecticide was observed. Although the two control strategies avert almost equal numbers of infections in the Pakistani region, this occurred as a result of the existence of a reciprocal relationship between insecticide cost and vaccination use [37]. Another modelling study that also described the minimum effort in mitigating dengue via suppressing the vector (female mosquito) population considered the production cost of SIT, insecticide application cost, and social (dengue disease-related) cost. They showed that the social cost is very important in reducing the female mosquito population and should be considered in controlling vectors responsible for transmitting dengue [62]. Further, researchers in [41] considered optimal control approaches for establishing Wolbachia-infected mosquitoes and compared two options: (a) the importance of both time and production cost of Wolbachia-infected mosquitoes; and (b) time is more important than the cost of production. Option (b) results in overpopulation of Wolbachia-infected mosquitoes as this is a negative side effect, while option (a) can annul the overpopulation effect as releases are suspended approximately 5.5 weeks earlier [41]. One study investigated mosquito reduction management and cost using temephos and fumigation. They showed that the most effective strategies in mitigating dengue burden with the cheapest cost when control was initiated with a small number of vectors together with a simultaneous combination of both temephos and fumigation control measures [63].
Some studies investigated optimal control strategies to avert disease burden [37,48,49,56,63] and the effect of seasonality [48,49,56]. A study investigated the optimal control strategies for insecticide spraying and the use of insecticide-treated bed nets (ITN) to mitigate human infections and intervention costs [48]. They showed that the most effective strategy in averting dengue infections is the combination of ITN and insecticide spraying. However, insecticide spraying alone (without additional ITN) should be implemented in areas of at least low seasonality, being both effective and the most cost beneficial. In the absence of seasonality (amplitude of seasonal force) for mild climate scenarios, ITN could not eliminate disease (within a year timeframe). However, combining ITN with insecticide spraying reduced the infection prevalence and led to no infection within five months. Wijaya and Gotz also investigated the application of optimal control models via two categories: chemical dissemination of aquatic mosquitoes (eggs and larvae) and fumigation of adult mosquitoes [63]. Results from numerical simulations suggest that, although maintaining fumigation instead of the use of chemicals, such as temephos, may be beneficial, combining the two control strategies most significantly reduced the vector (mosquito) population [63].
Another study, which sought to reveal two optimal timings at which pesticide is sprayed within the seasonal period in a year, investigated two optimization scenarios of pesticide spraying [49]. The first scenario described fixing the peak number of dengue-infected hosts at specific intervals and, afterwards, detecting the optimal timing through repetition of pesticide application timings that generates the minimum amounts of pesticide per application required. The second scenario inversely considered fixing the number of pesticides and minimising the dengue infection peak. It was shown via the first scenario that the optimal timing of the first pesticide application varies between 33–43 days, while the second remains approximately constant at 220 days before the peak of infection. However, the second scenario revealed that the optimal timing for the first pesticide application remains constant (around 28 days) while the second takes values between 232–281 days [49]. Two similar studies also investigated the optimal timing of insecticide fogging together with seasonality (where both wet and dry seasons were considered) [56,85]. The authors in [56] simulated four scenarios of the model, which include adding seasonality, endemic state, and different transmission intensities by systematically increasing the number of mosquitoes per person (that is, from low (2) to very high endemicity (15)). They concluded that the optimal timing of application oscillated between the beginning of the wet season (dengue season) and the prevalence peak [56]. This occurred because the timing could interfere with the exponentially growing epidemic. Further, researchers in [85] investigated the optimal timing of fogging, which includes the deployment of ultra-low volume (ULV) and targeted indoor residual spraying (TIRS), using different spraying strategies, such as yearly, biannually, or when the number of dengue cases exceeded the adaptive threshold of the average incidence. They used a simulation-based model to parameterize data from 2000 to 2010 in Iquitos, Peru. They showed, in general, TIRS has higher efficacy and averted more dengue infections than ULV. Of the different spraying strategies applied to both ULV and TIRS, the adaptive threshold strategy for TIRS is the most effective, with a 97% reduction in the number of infections from baseline and requiring fewer days of spraying (three quarters of a year) [85]. A sensitivity analysis was performed to explore how the adaptive threshold spraying strategies could be affected by delays in reporting or underreporting. They found that these delays do not affect the serotype-specific calibration of the model [85].
4.2. Biological Control Methods
Biological methods for vector control of dengue encompass the introduction of biological agents, such as small fishes, crustaceans, and bacteria [16,75,86]. These agents typically include larvivorous fishes [87,88], cyclopoid copepods [89,90], and Bacillus thuringiensis israelensis (BTI) [91,92,93]. Additionally, biological control methods may also include the alteration of the genetic materials of vectors, thereby inhibiting them from transmitting the dengue virus [16]. This subclass includes sterile insect techniques (SIT) [94,95], genetically modified mosquito (GMM) methods [96,97], such as the release of insects carrying a dominant lethal (RIDL) gene [96,98] and Wolbachia bacterium introduction (WI) [15,22,23,29,99].
Prior to formulating models to biologically control vectors fuelling the transmission of dengue, it is worth mentioning, in general, some factors to be considered in governing model interests and initiation. These factors include describing the biological agents (vectors) to be used [16,36,49,53,86,88], understanding ecological patterns between the vector and dengue virus [15,83,100], and identifying the methods of control [15,29,67,95,96]. Different model structures account for the biological vectors used by modelling vector-only transmission dynamics involving the dengue virus [29,40,64]. These models account for the competitive interaction between wild-type and biologically infected vectors, in particular, mosquitoes [38,42]. Of the three factors, the ecological patterns between the vector and the virus can be modelled using human–vector transmission models [52,57,101], which capture the interaction between the viral-infected mosquitoes and uninfected humans and vice versa. These control methods are considered by incorporating a control type, such as Wolbachia-based control, that may consider complex features, such as CI and IMT effects in vectors [35,95,98,99]. These are some of the complexities in model structures used for different forms of biological controls.
Dengue models formulated by investigating the effects of the biological methods of vector control are described in 19 studies [32,34,35,38,40,41,42,43,44,50,51,52,53,55,57,58,62,64,65]. Except for one [55], which is a network model (NM), all of the other 18 studies use deterministic models (DM). Of all the 19 modelling studies, seven articles [35,38,42,43,52,55,57] model the interaction between human and vector populations, while 12 studies [32,34,40,41,44,50,51,53,58,62,64,65] model the vector population dynamics, where the vector population in all cases is considered in the presence of a biological control mechanism, such as SIT, GMM, or Wolbachia introductions. Presently, the biological method of dengue vector control is the most commonly modelled and analysed as compared with about a decade ago (prior to the successful introduction of some biological techniques, such as WI), when mostly chemical control methods were considered [66].
Different studies have recognised key determinants of success-mating competitiveness of SIT versus wild-type mosquitoes in combination with other control methods and recruitment and release rates to control dengue viral infection [32,34,40,55,57,62]. These DM of SIT studies [32,34,40,62] model vector population dynamics and investigate release rates and sizes. Another DM study [57] considered both vector and vector–human population dynamics, and one NM study [55] only described human–vector population dynamics. These models involved state variables which may include young and adult sex-structured vector populations. One similar study assumed that the male mortality rate is higher than that of the female [32]. These studies considered constant [32,34,40] and periodic [32,34,62] releases of sterile insects to achieve elimination. For the constant releases (usually sterile males), the number of sterile mosquitoes released at the initial stage of the release timeframe is constant. This demonstrates that every solution of the system tends to an equilibrium point (especially disease-free equilibrium) for the constant release of sterile mosquitoes, even in the presence of a time delay in the developmental stage of the uninfected mosquitoes [34,40]. For periodic releases, control is achieved at a lesser cost compared to constant release control [34].
A study [40], which modelled the interactive competitiveness between wild-type and sterile mosquitoes, considered and analysed the delay in time to releasing sterile mosquitoes. They showed that the delay imposed while releasing the sterile mosquitoes at a constant rate does not significantly affect the system dynamics. However, if both wild-type and sterile mosquitoes are released at the same rate, there is a profound effect on the system dynamics, especially as the delay in release time increases as a result of Hopf bifurcations [40]. In contrast to constant release, delay in periodic releases of sterile males (i.e., release rate proportional to the wild mosquito population) may greatly affect the system dynamics. As the time delay increases, the system’s solution may show an oscillatory behaviour through Hopf bifurcations. At this point, both the sterile and wild mosquito populations can coexist [40].
Several SIT control approaches require sterile mosquitoes to compete almost equally with their wild counterparts to be effective, as their effectiveness may depend on the size of the wild populations [34]. The study [34] further suggested that the mating competitiveness of the SIT control method should tend to one (as good as the wild-type) to boost effectiveness. Otherwise, the SIT efficacy may diminish, provided there are existing wild-type mosquitoes. Another study [57] showed that when the SIT is supplemented with pupicide pyriproxifen (PP), it could increase the effectiveness of the intervention by averting over 95% of the total rollout and, in turn, decrease the dengue burden. Additionally, a network model [55] revealed that SIT application could be successful depending on the rate of recruitment and coupling strength of the migration parameter.
The modelling of genetically modified mosquitoes (GMM), such as the release of insects carrying dominant lethal (RIDL) methods, are analysed in three studies [38,58,64]. A dynamic model that accounts for the RIDL release of pupal and adult mosquitoes was unveiled via simulations that, for regularly recurring releases, the most effective RIDL approach is evident when only adult-carrying RIDL mosquitoes are released every day [64]. The adult-only RIDL mosquito approach outperforms both pupal and combined mosquitoes’ releases because the adult male RIDL mosquitoes are already sexually matured and, as such, would perform well in increasingly maintaining the RIDL mosquitoes after release until the next day’s release. Unlike adult RIDL releases, pupal-only RIDL releases would require that the pupae gradually develop into adult males and therefore are affected by high mortality between the pupa to sexually active adult time, causing a disadvantage. Whereas, for the long-term suppression of wild population scenarios with infrequent RIDL releases, the combination of pupal and adult mosquitoes’ release could maintain and sustain suppression every week when compared with pupal- or adult-only releases. Similarly, about 1.9 million combined mosquitoes’ release (73% pupae and 27% adults) was able to maintain suppression, while pupae- or adult-only mosquitoes’ release could maintain suppression if the population sizes were increased to 2.7 and 2.8 million, respectively [64]. Further, another model considered a GMM “reduce and replace” (RR) technique that introduced insects possessing genetic features, which included female-killing and antipathogenic attributes [58]. The authors showed that the continuous release of RR mosquitoes resulted in a long-term decrease in the overall density of the vectors (mosquitoes) [58]. When a proportion of RR male-only mosquitoes were released for a year, the population density of the adult female mosquitoes decreased with a more rapid reduction in the density of the competent vectors than the population density of the total female mosquitoes. The competent vector density decreased rapidly due to an increase in the frequency of the antipathogenic allele. However, when the release ceased, the female population recovered to its initial size, but the competent vector remained at an insignificantly low density [58]. Considering the release of RR female mosquitoes and comparing with male-only and both-sex mosquito releases for 100 days with a release ratio of one, the female-only releases mostly reduced the total adult female wild population. Although the total female population surged initially as a result of releasing more RR females, the total density of adult females was effectively reduced for longer periods of time. Concisely, it was shown that suppressing the vector population density would be dependent on release proportion and duration and adult female mosquitoes’ inclusion in the GMM releases [58]. Increasing the fitness cost associated with the antipathogenic gene for a year simulation of male-only RR rollout at a release ratio of two led to a reduction in the competing vector density [58]. Modelling the effect of releasing RIDL from the cost-effectiveness perspective [38] showed that the RIDL control technique could quickly eradicate dengue at a low cost and was, therefore, highly cost-effective.
From the study articles selected for this review and then stratified into biological vector control so far, Wolbachia control strategies are the most modelled and have been analysed to inform the effective control of Aedes mosquito vectors to mitigate dengue burden [35,41,42,43,44,50,51,52,53,65]. Wolbachia-based control is the introduction of the intracellular bacterium Wolbachia into arthropods to suppress vector populations, disrupt arboviral transmission, or both [29]. Wolbachia infection is transmitted maternally (that is, from the adult female arthropod to the offspring). There are various strains of Wolbachia, such as wAu, wMel, and wPip, amongst others. Wolbachia possess some features that may depend on the strains, such as uni- or bi-directional cytoplasmic incompatibility (CI), the phenomenon that causes incompatibility between the sperms and eggs of arthropods (mosquitoes) resulting in unviable offspring; imperfect maternal transmission (IMT); viral blockage; Wolbachia infection loss; and mosquito fitness cost [29]. Sex-structured models accounting for the interactive competitiveness of wild-type and Wolbachia-infected mosquitoes were described in [41,44,53,65]. Some models have investigated Wolbachia-carrying mosquito features, such as fitness effects, IMT, viral blockage, CI, and Wolbachia loss [30,41,42,45,51,65]. These features have been suggested to affect the spread, establishment, and dominance of Wolbachia infections in mosquitoes [30,45,101]. One study showed that the evolution of a complete CI could drive the successful invasion of Wolbachia in a wild-type mosquito population; however, incomplete CI by genetic evolution may compromise successful invasion [51]. In other words, the authors revealed that the successful establishment or failure of Wolbachia-infected mosquitoes might rely on the selected Wolbachia strain [51].
Other human–vector dynamical models in the presence of Wolbachia have been analysed as these models, together with experimental data, have provided insights into how the presence of Wolbachia-infected mosquito rollouts have significantly reduced dengue disease [35,42,43,50,52]. One of these studies [43], focusing on dengue infection and Wolbachia-infected mosquito rollout dynamics in Indonesia, used the combination of multiple modelling methods together with available data from Indonesia to show that approximately 7.8 million dengue cases were estimated to be symptomatic in 2015. However, this analysis may be an overestimation as it is highly sensitive to the assumed under-reporting rate, where about five million cases were estimated to have individually managed the symptoms via informal healthcare services. Additionally, of the total estimated symptomatic cases, only 14.1% were estimated to have been hospitalized, resulting in over three thousand deaths [43]. The researchers in [43] also estimated that the Wolbachia rollout program conducted in Indonesia averted 86.2% of dengue cases over a year. Similarly, another modelling article used an estimated transmission rate of 0.1648 new human transmissions per dengue-infected mosquito per day by fitting a deterministic model to experimental data from a northern Queensland city, Cairns, in Australia. The authors estimated an 80% decrease in overall dengue cases after a Wolbachia rollout [42]. Further, they showed that for weekly introductions of Wolbachia in Cairns, half of the dengue cases were reduced for a year, while about 60% were reduced for quarterly time periods. The researchers in [42] further showed that the duration of dengue outbreaks could be decreased by between 2 and 6 weeks yearly in the presence of Wolbachia-infected mosquito rollouts based on the seasonality strength. This decrease may have been caused by a reduction in the mosquito’s lifespan [42]. The study [52] also described modelling the use of Wolbachia for dengue control. They showed that infecting Aedes mosquitoes with Wolbachia bacteria decreased the basic reproductive number for dengue virus and, in particular, for the wAlbB Wolbachia strain, the reproductive number is reduced by around two-thirds, which would be sufficient to prevent epidemic outbreaks [52].
4.3. Environmental Control Methods
Environmental control programs focus on the reduction of mosquito breeding and reproduction via the media of modification to the surrounding environment. These media include installing efficient piped water supplies and good drainage systems; emptying, covering, or destroying stagnant waterlogged cans and containers; practising proper environmental hygiene (cleaning of the environment such as mosquito breeding sites); and implementing waste management schemes. Additionally, environmental factors, such as seasonal variation and changes in temperature, may also serve as environmental modifications of vectors to mitigate their abundance. Of all the vector control methods, environmental control does not pose environmental contamination risks as it predominantly entails common hygienic practices and maintenance, addressing seasonal fluctuations in cases. Its impact can be lifelong and does not require further investments for sustainability.
Mathematical models of environmental control studies have sparsely been formulated as these models are not often described (in just three of the selected articles) [39,59,60]. The deterministic models in [39,59] showed that seasonal variations could affect the dengue epidemic dynamics; that is, autumn and summer seasons could greatly increase dengue transmission in the presence of an infectious individual within a short time period [59]. This suggests that large outbreaks of dengue could have been fuelled by warm temperatures [59]. A model [39] that considered seasonal variations via periodic forcing in the vector density and the impact of vector control methods in the 2005 Singapore dengue outbreak estimated the basic reproductive number to be 1.363 [39]. The authors showed that dengue infection would not persist except if the recruitment rate is more than the ratio of the periodic vector recruitment rate with a yearly period to the square of the basic reproductive number [39]. This showed that the basic reproduction number, under periodic environment (or asymptotic behaviour of the system—bifurcation), described the threshold for disease persistence. They also revealed that the dengue incidence, which occurred in the 10th month of each year (2003–2005), was described by a lag of 4.2 months with the highest mosquito density [39]. Similarly, another model, together with experimental data from Funchal, Madeira Island, accounts for seasonality via varying temperature over time by periodic forcing in the dengue transmission in Madeira Island, Portugal [59]. Considering the different simulated arrival dates of an infectious individual into the population of the uninfected/susceptible, it was revealed that an epidemic outbreak is expected to occur between July and November each year [59]. Therefore, with an infected individual arrival time in August and October, the shortest and longest epidemic time simulated was 93 days and 411 days, respectively. For the shortest epidemic time, approximately one-tenth of the susceptible population was infected, while 3.4% of susceptibles were infected in the longest epidemic time [59]. A general multi-patch model of dengue dynamics together with experimental data from Kolkata, India, revealed that control methods with higher environmental persistence, such as the treatment of surface and materials (TSM), mostly decreased dengue cases as compared with the use of ultra-low volume (ULV) spray of insecticides and lethal ovitraps (LO) [60]. Specifically, the comparison between the single applications of the three strategies: the use of ULV, LO, and TSM showed reductions of 2.9%, 48%, and 49.1%, respectively, with TSM ranking highest. Considering pairwise and three-way comparisons of the control methods, any combination with TSM ranked highest as the three-way combination reduced 72.7% of the total cumulative cases [60]. In all, the above review suggests that environmental vector control modelling studies have lots of potential but are currently under-investigated, and, therefore, more modelling studies need to be conducted to account for the environmental vector control impacts towards the eradication of dengue.
4.4. Quality Assessment of Study Results
The selected studies possessed an Assessment of Modelling Studies (AMS) score range from 66.67–91.67% (Table 3). Thus, all scored at least a ‘High’ methodological quality (cut-off for high is 65%). Additionally, of the 32 studies included, 13 scored above 80%, as these studies fell into the ‘Very High’ category on the Assessment of Study Quality (ASQ). In all, the selected studies provided in detail the description of model structure, methods and validation, parameter specifications, assumptions made, intervention comparators and quality of data, and uncertainty/sensitivity analysis.
Table 3.
Table showing the distribution of study quality with respect to the vector control types.
To further investigate if there was a difference in the quality of the studies (Very High and High) across the different vector control methods (chemical, biological, and environmental), a bivariate analysis was performed using Fisher’s exact test. Our analysis showed that there is no significant difference in the study quality (Very High and High) of the different vector control methods (p = 0.4). In other words, there is no statistically significant difference in the proportion of ‘High’ versus ‘Very High’ quality studies across the vector controls (Figure 4). Given the relatively small number of studies investigating environmental control (3 out of 32), the ‘High’ rating assigned to this category should be interpreted with caution.
Figure 4.
Mozaic plot showing the distribution of the bounded area of study quality of the vector control types.
5. Discussion
The mathematical modelling of dengue transmission can be useful in understanding disease dynamics [102,103,104]. It is a significant tool that can assist in predicting and curtailing outbreaks of dengue disease and help in reducing transmission of infection and mitigating the dengue burden [35,42,47,54,59,60]. Overall, our study reviews the effectiveness of mathematical modelling of different vector control approaches to reduce the spread of dengue disease. In this review, we identified 32 articles that met our search criteria. We then stratified the selected articles into the modelling types: deterministic, stochastic and network modelling methods. The articles mainly consisted of deterministic modelling methods for dengue vector control (88% of the total selected studies). Other modelling approaches, such as stochastic and network modelling, shared 9% and 3% of the total selected studies, respectively. Based on the vector control approaches, we grouped the selected articles into three vector control approaches: chemical (11), biological (18), and environmental (3).
Modelling studies demonstrate that the chemical vector control methods, such as the use of insecticides for outdoor fogging or indoor residual spraying, insecticide-treated bed nets (ITN), insecticide-treated house screens (ITHS), and insecticide-treated door curtains (ITC) for dengue transmission, could be highly effective in reducing the burden of dengue when scaled up [33,46,49,56]. They also showed that when the dengue burden is high, chemical controls are best used in combination, while a single control technique, such as insecticide spraying, may be adequate for areas with low endemicity [48]. One important prediction from modelling is that long-time usage of this method could fuel mosquitoes’ resistance to the chemicides and then result in a less effective and efficient control strategy [54]. These modelling results need to be considered in addition to the known threat to the environment via contaminating water bodies and air pollution [16].
On the other hand, biological vector control methods are gaining global popularity and usage as some of these methods are self-sustaining [29,30]. Accordingly, various mathematical models accounting for the biological control of vectors to mitigate dengue spread have been formulated in the last decades [32,34,40,55,57,62]. These modelling studies consider the transmission dynamics of releasing sterile insect techniques (SIT), genetically modified mosquitoes (GMM) and Wolbachia-infected mosquitoes (among other interventions) to curb the spread of dengue infection. Our review has presented an understanding of SIT techniques and how they could be very effective in controlling dengue infection; however, when boosted with pupicide pyriproxifen (PP), they could greatly reduce the number of sterile males required to eliminate the mosquito population [57]. This could only be established in areas with high but not low mosquito densities. According to a network model, SIT could be very effective in reducing dengue viral infection as that would depend on the rate of recruiting sterile mosquitoes, migration parameters and coupling effect [55]. For GMM methods, such as RIDL techniques, which could be less expensive to conduct [38], the effectiveness of these methods could depend on the proportion of RIDL release, duration of release, and, most especially, the inclusion of adult-RIDL female mosquitoes [58].
Wolbachia-infected mosquito rollouts have been very effective in averting dengue cases, with an estimated reduction of over 80% in countries such as Indonesia and Australia [42,43]. Since then, there have been increasing numbers of models addressing transmission dynamics and features that drive successful strategies, with 10 of the 18 models on biological methods focused on Wolbachia-based mosquito control. The effectiveness of Wolbachia-carrying mosquitoes is dependent on reproductive advantage CI, fitness effect, maternal transmission, and viral blocking strength [22]. Furthermore, Wolbachia-infected mosquito release programs could also decrease the duration of feasible outbreaks of dengue infection by a month and a half [43].
Regarding the mathematical modelling of environmental control methods, there are few articles describing the modelling impact. Although some of these models are conjoined with other control methods, such as chemical and biological methods, model outcomes suggest that environmental interventions—for instance, treating surfaces and materials and seasonal variations could have a greater impact in reducing dengue cases when compared to chemical methods, such as insecticide spraying without the attendant environmental contamination [39,59,60]. This sparse modelling work is encouraging, and future studies on environmental actions alone and in combination with other control measures are needed.
Strengths and Limitations
This review relied on the modelling results of articles taken from the extensive database search describing the vector controls of dengue transmission dynamics models. These models showcased the different control techniques in mitigating dengue viral transmission. As far as the authors are aware, this review is the first to explore the present understanding of vector control approaches and the effective role of mathematical models in mitigating or eliminating dengue. However, the selected articles were not evenly distributed as more than half of the studies were from 2017 onwards (Figure 3). This may have been a consequence of the severe dengue outbreaks in the Americas, and some parts of South East Asian region from 2018 to 2019, arousing interest in vector control and modelling studies [71]. Further, only published English journal articles were considered as non-English studies were excluded to avoid oversight. Other referencing types, such as book sections, conference proceedings, and serials, were excluded as they did not contain sufficient detail to assess the studies. In addition, the other referencing types are approximately 3% of the searched articles after removing the duplicates, and, as such, their exclusion has an insignificant impact. We have only considered dengue transmission models via three major control types (chemical, biological, and environmental) in this work. Of these control types, environmental control studies constitute relatively few (9% of the selected studies) and that would have had an impact on the results, possibly creating some biases in the evaluation. Although there is an emerging control method, mechanical control, mathematical models are still sparsely formulated and analysed in this regard. Essentially, the AMS tool used in appraising the included articles relies in part on the authors’ knowledge and, as such, could create grounds for possible bias [69]. Overall, there is a chance for information bias as some articles may not have been included in the databases used for this research study.
6. Conclusions
In summary, our study, based on the selected published articles, provided a detailed understanding of all three methods of vector controls and their effectiveness. However, the magnitude of their effectiveness has some dependencies. The chemical method has some drawbacks based on the evolution of vector resistance resulting in decreased efficacy of these methods. The biological method could be a self-sustaining form of control as trans-infected mosquitoes (with Wolbachia) could pass on the Wolbachia infections to the offspring, thereby, inhibiting the transmission of dengue. This has been shown to be very effective; however, factors such as seasonality and heatwaves could reduce the effectiveness through loss of Wolbachia infection in mosquitoes. Environmental control methods have lots of potential but are currently under-investigated; therefore, there is a need to further model environmental parameters, such as healthy drainage systems, covering of water containers, and good hygiene, to inform the impact on the dengue burden. In all, there is a strong need to consider the combination of the three methods of vector control via mathematical modelling studies to evaluate the impact on the eradication or elimination of dengue disease at large.
Supplementary Materials
The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/v15010254/s1. Additional File S1: Search Strategies for Systematic Review.
Author Contributions
Conceptualization, S.T.O. and E.S.M.; methodology, S.T.O., E.S.M. and M.T.M.; software, S.T.O., E.S.M., M.T.M. and A.I.A.; validation, S.T.O., E.S.M., M.T.M. and A.I.A.; investigation, S.T.O.; resources, S.T.O., E.S.M., M.T.M. and A.I.A.; data curation, writing—original draft preparation, S.T.O.; writing—reviewing and editing, S.T.O., E.S.M., M.T.M. and A.I.A.; supervision, E.S.M., M.T.M. and A.I.A.; project administration, E.S.M.; funding acquisition, E.S.M. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Acknowledgments
The authors of this paper gratefully acknowledge the James Cook University Postgraduate Research Scholarship (JCUPRS), Queensland, Australia, awarded to STO (PhD scholarship), College of Medicine and Dentistry, College of Public Health, Medical and Veterinary Sciences and Australian Institute of Tropical Health and Medicine (AITHM), James Cook University, Australia.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Guzman, M.G.; Harris, E. Dengue. Lancet 2015, 385, 453–465. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gould, E.; Pettersson, J.; Higgs, S.; Charrel, R.; De Lamballerie, X. Emerging arboviruses: Why today? One Health 2017, 4, 1–13. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bhatt, S.; Gething, P.W.; Brady, O.J.; Messina, J.P.; Farlow, A.W.; Moyes, C.L.; Drake, J.M.; Brownstein, J.S.; Hoen, A.G.; Sankoh, O.; et al. The global distribution and burden of dengue. Nature 2013, 496, 504–507. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Buhler, C.; Winkler, V.; Runge-Ranzinger, S.; Boyce, R.; Horstick, O. Environmental methods for dengue vector control—A systematic review and meta-analysis. PLoS Negl. Trop. Dis. 2019, 13, e0007420. [Google Scholar] [CrossRef] [Scilit]
- Simmons, C.P.; Farrar, J.J.; van Vinh Chau, N.; Wills, B. Dengue. N. Engl. J. Med. 2012, 366, 1423–1432. [Google Scholar] [CrossRef] [Scilit]
- Reich, N.G.; Shrestha, S.; King, A.; Rohani, P.; Lessler, J.; Kalayanarooj, S.; Yoon, I.-K.; Gibbons, R.V.; Burke, D.S.; Cummings, D.A.T. Interactions between serotypes of dengue highlight epidemiological impact of cross-immunity. J. R. Soc. Interface 2013, 10, 20130414. [Google Scholar] [CrossRef] [Scilit]
- Fukusumi, M.; Arashiro, T.; Arima, Y.; Matsui, T.; Shimada, T.; Kinoshita, H.; Arashiro, A.; Takasaki, T.; Sunagawa, T.; Oishi, K. Dengue Sentinel Traveler Surveillance: Monthly and Yearly Notification Trends among Japanese Travelers, 2006–2014. PLoS Negl. Trop. Dis. 2016, 10, e0004924. [Google Scholar] [CrossRef] [Scilit]
- Capeding, M.R.; Tran, N.H.; Hadinegoro, S.R.S.; Ismail, H.I.H.M.; Chotpitayasunondh, T.; Chua, M.N.; Luong, C.Q.; Rusmil, K.; Wirawan, D.N.; Nallusamy, R.; et al. Clinical efficacy and safety of a novel tetravalent dengue vaccine in healthy children in Asia: A phase 3, randomised, observer-masked, placebo-controlled trial. Lancet 2014, 384, 1358–1365. [Google Scholar] [CrossRef] [Scilit]
- Villar, L.; Dayan, G.H.; Arredondo-García, J.L.; Rivera, D.M.; Cunha, R.; Deseda, C.; Reynales, H.; Costa, M.S.; Morales-Ramírez, J.O.; Carrasquilla, G.; et al. Efficacy of a Tetravalent Dengue Vaccine in Children in Latin America. N. Engl. J. Med. 2015, 372, 113–123. [Google Scholar] [CrossRef] [Scilit]
- Wilder-Smith, A.; Ooi, E.-E.; Horstick, O.; Wills, B. Dengue. Lancet 2019, 393, 350–363. [Google Scholar] [CrossRef] [Scilit]
- Sulistyawati, S.; Astuti, F.D.; Umniyati, S.R.; Satoto, T.B.T.; Lazuardi, L.; Nilsson, M.; Rocklov, J.; Andersson, C.; Holmner, A. Dengue Vector Control through Community Empowerment: Lessons Learned from a Community-Based Study in Yogyakarta, Indonesia. Int. J. Environ. Res. Public Health 2019, 16, 13. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Otu, A.; Ebenso, B.; Etokidem, A.; Chukwuekezie, O. Dengue fever-an update review and implications for Nigeria, and similar countries. Afr. Health Sci. 2019, 19, 2000–2007. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ferguson, N.M. Challenges and opportunities in controlling mosquito-borne infections. Nature 2018, 559, 490–497. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wilder-Smith, A.; Vannice, K.S.; Hombach, J.; Farrar, J.; Nolan, T. Population Perspectives and World Health Organization Recommendations for CYD-TDV Dengue Vaccine. J. Infect. Dis. 2016, 214, 1796–1799. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tatuene, J.K.; Makepeace, B.L.; Benjamin, L.; Baylis, M.; Solomon, T. The potential role of Wolbachia in controlling the transmission of emerging human arboviral infections. Curr. Opin. Infect. Dis. 2017, 30, 108–116. [Google Scholar] [CrossRef] [Scilit]
- Horstick, O.; Boyce, R.; Runge-Ranzinger, S. Dengue Vector Control: Assessing What Works? Southeast Asian J. Trop Med. 2017, 48, 181–195. [Google Scholar]
- Dusfour, I.; Vontas, J.; David, J.-P.; Weetman, D.; Fonseca, D.M.; Corbel, V.; Raghavendra, K.; Coulibaly, M.B.; Martins, A.J.; Kasai, S.; et al. Management of insecticide resistance in the major Aedes vectors of arboviruses: Advances and challenges. PLoS Negl. Trop. Dis. 2019, 13, e0007615. [Google Scholar] [CrossRef] [Scilit]
- Loroño-Pino, M.A.; Chan-Dzul, Y.N.; Zapata-Gil, R.; Carrillo-Solís, C.; Uitz-Mena, A.; García-Rejón, J.E.; Keefe, T.J.; Beaty, B.J.; Eisen, L. Household use of insecticide consumer products in a dengue-endemic area in México. Trop. Med. Int. Health 2014, 19, 1267–1275. [Google Scholar] [CrossRef] [Scilit]
- Lacroix, R.; McKemey, A.R.; Raduan, N.; Kwee Wee, L.; Hong Ming, W.; Guat Ney, T.; Rahidah, A.A.S.; Salman, S.; Subramaniam, S.; Nordin, O.; et al. Open Field Release of Genetically Engineered Sterile Male Aedes aegypti in Malaysia. PLoS ONE 2012, 7, e42771. [Google Scholar] [CrossRef] [Scilit]
- Carvalho, D.O.; McKemey, A.R.; Garziera, L.; Lacroix, R.; Donnelly, C.A.; Alphey, L.; Malavasi, A.; Capurro, M.L. Suppression of a Field Population of Aedes aegypti in Brazil by Sustained Release of Transgenic Male Mosquitoes. PLoS Negl. Trop. Dis. 2015, 9, e0003864. [Google Scholar] [CrossRef] [Scilit]
- Lebon, C.; Benlali, A.; Atyame, C.; Mavingui, P.; Tortosa, P. Construction of a genetic sexing strain for Aedes albopictus: A promising tool for the development of sterilizing insect control strategies targeting the tiger mosquito. Parasites Vectors 2018, 11, 658. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ant, T.H.; Herd, C.S.; Geoghegan, V.; Hoffmann, A.A.; Sinkins, S.P. The Wolbachia strain wAu provides highly efficient virus transmission blocking in Aedes aegypti. PLoS Pathog. 2018, 14, e1006815. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mohanty, I.; Rath, A.; Mahapatra, N.; Hazra, R.K. Wolbachia: A biological control strategy against arboviral diseases. J. Vector Borne Dis. 2016, 53, e1006815. [Google Scholar]
- Hoffmann, A.A.; Montgomery, B.L.; Popovici, J.; Iturbeormaetxe, I.; Johnson, P.H.; Muzzi, F.; Greenfield, M.; Durkan, M.; Leong, Y.S.; Dong, Y.; et al. Successful establishment of Wolbachia in Aedes populations to suppress dengue transmission. Nature 2011, 476, 454–457. [Google Scholar] [CrossRef] [Scilit]
- Barrera, R. New tools for Aedes control: Mass trapping. Curr. Opin. Insect Sci. 2022, 52, 100942. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hemme, R.R.; A Smith, E.; Felix, G.; White, B.J.; I Diaz-Garcia, M.; Rodriguez, D.; Ruiz-Valcarcel, J.; Acevedo, V.; Amador, M.; Barrera, R. Multi-Year Mass-Trapping with Autocidal Gravid Ovitraps has Limited Influence on Insecticide Susceptibility in Aedes aegypti (Diptera: Culicidae) from Puerto Rico. J. Med. Èntomol. 2022, 59, 314–319. [Google Scholar] [CrossRef] [Scilit]
- Jahir, A.; Kahamba, N.F.; Knols, T.O.; Jackson, G.; Patty, N.F.A.; Shivdasani, S.; Okumu, F.O.; Knols, B.G.J. Mass Trapping and Larval Source Management for Mosquito Elimination on Small Maldivian Islands. Insects 2022, 13, 805. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lana, R.M.; Morais, M.M.; De Lima, T.F.M.; Carneiro, T.; Stolerman, L.M.; Dos Santos, J.P.C.; Cortês, J.J.C.; Eiras, E.; Codeço, C.T. Assessment of a trap based Aedes aegypti surveillance program using mathematical modeling. PLoS ONE 2018, 13, e0190673. [Google Scholar] [CrossRef] [Scilit]
- Ogunlade, S.; Meehan, M.; Adekunle, A.; Rojas, D.; Adegboye, O.; McBryde, E. A Review: Aedes-Borne Arboviral Infections, Controls and Wolbachia-Based Strategies. Vaccines 2021, 9, 32. [Google Scholar] [CrossRef] [Scilit]
- Adekunle, A.I.; Meehan, M.T.; McBryde, E.S. Mathematical analysis of a Wolbachia invasive model with imperfect maternal transmission and loss of Wolbachia infection. Infect. Dis. Model. 2019, 4, 265–285. [Google Scholar] [CrossRef] [Scilit]
- Almeida, L.; Privat, Y.; Strugarek, M.; Vauchelet, N. Optimal Releases for Population Replacement Strategies: Application to Wolbachia. SIAM J. Math. Anal. 2019, 51, 3170–3194. [Google Scholar] [CrossRef] [Scilit]
- Bliman, P.-A.; Cardona-Salgado, D.; Dumont, Y.; Vasilieva, O. Implementation of control strategies for sterile insect techniques. Math. Biosci. 2019, 314, 43–60. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marini, G.; Guzzetta, G.; Toledo, C.A.M.; Teixeira, M.; Rosà, R.; Merler, S. Effectiveness of Ultra-Low Volume insecticide spraying to prevent dengue in a non-endemic metropolitan area of Brazil. PLoS Comput. Biol. 2019, 15, e1006831. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Strugarek, M.; Bossin, H.; Dumont, Y. On the use of the sterile insect release technique to reduce or eliminate mosquito populations. Appl. Math. Model. 2019, 68, 443–470. [Google Scholar] [CrossRef] [Scilit]
- Zhang, H.; Lui, R. Releasing Wolbachia-infected Aedes aegypti to prevent the spread of dengue virus: A mathematical study. Infect. Dis. Model. 2020, 5, 142–160. [Google Scholar] [CrossRef] [Scilit]
- Andraud, M.; Hens, N.; Marais, C.; Beutels, P. Dynamic Epidemiological Models for Dengue Transmission: A Systematic Review of Structural Approaches. PLoS ONE 2012, 7, e49085. [Google Scholar] [CrossRef] [Scilit]
- Agusto, F.; Khan, M. Optimal control strategies for dengue transmission in pakistan. Math. Biosci. 2018, 305, 102–121. [Google Scholar] [CrossRef] [Scilit]
- Alphey, N.; Alphey, L.; Bonsall, M.B. A Model Framework to Estimate Impact and Cost of Genetics-Based Sterile Insect Methods for Dengue Vector Control. PLoS ONE 2011, 6, e25384. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Andraud, M.; Hens, N.; Beutels, P. A simple periodic-forced model for dengue fitted to incidence data in Singapore. Math. Biosci. 2013, 244, 22–28. [Google Scholar] [CrossRef] [Scilit]
- Cai, L.; Ai, S.; Fan, G. Dynamics of delayed mosquitoes populations models with two different strategies of releasing sterile mosquitoes. Math. Biosci. Eng. 2018, 15, 1181–1202. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Campo-Duarte, D.E.; Vasilieva, O.; Cardona-Salgado, D.; Svinin, M. Optimal control approach for establishing wMelPop Wolbachia infection among wild Aedes aegypti populations. J. Math. Biol. 2018, 76, 1907–1950. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ndii, M.Z.; Allingham, D.; Hickson, R.; Glass, K. The effect of Wolbachia on dengue outbreaks when dengue is repeatedly introduced. Theor. Popul. Biol. 2016, 111, 9–15. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- O’Reilly, K.M.; Hendrickx, E.; Kharisma, D.D.; Wilastonegoro, N.N.; Carrington, L.B.; Elyazar, I.R.F.; Kucharski, A.J.; Lowe, R.; Flasche, S.; Pigott, D.M.; et al. Estimating the burden of dengue and the impact of release of wMel Wolbachia-infected mosquitoes in Indonesia: A modelling study. BMC Med. 2019, 17, 172. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qu, Z.; Xue, L.; Hyman, J.M. Modeling the Transmission of Wolbachia in Mosquitoes for Controlling Mosquito-Borne Diseases. SIAM J. Appl. Math. 2018, 78, 826–852. [Google Scholar] [CrossRef] [Scilit]
- Ogunlade, S.T.; Adekunle, A.I.; Meehan, M.T.; Rojas, D.P.; McBryde, E.S. Modeling the potential of wAu-Wolbachia strain invasion in mosquitoes to control Aedes-borne arboviral infections. Sci. Rep. 2020, 10, 16812. [Google Scholar] [CrossRef] [Scilit]
- Abad-Franch, F.; Zamora-Perea, E.; Luz, S.L.B. Mosquito-Disseminated Insecticide for Citywide Vector Control and Its Potential to Block Arbovirus Epidemics: Entomological Observations and Modeling Results from Amazonian Brazil. PLoS Med. 2017, 14, e1002213. [Google Scholar] [CrossRef] [Scilit]
- Barmak, D.H.; Dorso, C.O.; Otero, M.; Solari, H.G. Modelling interventions during a dengue outbreak. Epidemiol. Infect. 2014, 142, 545–561. [Google Scholar] [CrossRef] [Scilit]
- Buonomo, B.; Della Marca, R. Optimal bed net use for a dengue disease model with mosquito seasonal pattern. Math. Methods Appl. Sci. 2018, 41, 537–592. [Google Scholar] [CrossRef] [Scilit]
- Chávez, J.P.; Götz, T.; Siegmund, S.; Wijaya, K.P. An SIR-Dengue transmission model with seasonal effects and impulsive control. Math. Biosci. 2017, 289, 29–39. [Google Scholar] [CrossRef] [Scilit]
- Hancock, P.A.; White, V.L.; Ritchie, S.A.; Hoffmann, A.A.; Godfray, H.C.J. Predicting Wolbachia invasion dynamics in Aedes aegypti populations using models of density-dependent demographic traits. BMC Biol. 2016, 14, 96. [Google Scholar] [CrossRef] [Scilit]
- He, S.; Zhang, X.; Liang, J.; Tang, S. Multiscale modelling the effects of CI genetic evolution in mosquito population on the control of dengue fever. Sci. Rep. 2017, 7, 13895. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hughes, H.; Britton, N.F. Modelling the Use of Wolbachia to Control Dengue Fever Transmission. Bull. Math. Biol. 2013, 75, 796–818. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, Y.; Liu, X. A sex-structured model with birth pulse and release strategy for the spread of Wolbachia in mosquito population. J. Theor. Biol. 2018, 448, 53–65. [Google Scholar] [CrossRef] [Scilit]
- Luz, P.M.; Vanni, T.; Medlock, J.; Paltiel, A.D.; Galvani, A.P. Dengue vector control strategies in an urban setting: An economic modelling assessment. Lancet 2011, 377, 1673–1680. [Google Scholar] [CrossRef] [Scilit]
- Aziz-Alaoui, M.A.; Gakkhar, S.; Ambrosio, B.; Mishra, A. A network model for control of dengue epidemic using sterile insect technique. Math. Biosci. Eng. 2018, 15, 441–460. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Oki, M.; Sunahara, T.; Hashizume, M.; Yamamoto, T. Optimal Timing of Insecticide Fogging to Minimize Dengue Cases: Modeling Dengue Transmission among Various Seasonalities and Transmission Intensities. PLoS Negl. Trop. Dis. 2011, 5, e1367. [Google Scholar] [CrossRef] [Scilit]
- Pleydell, D.R.J.; Bouyer, J. Biopesticides improve efficiency of the sterile insect technique for controlling mosquito-driven dengue epidemics. Commun. Biol. 2019, 2, 201. [Google Scholar] [CrossRef] [Scilit]
- Robert, M.A.; Okamoto, K.; Lloyd, A.L.; Gould, F. A Reduce and Replace Strategy for Suppressing Vector-Borne Diseases: Insights from a Deterministic Model. PLoS ONE 2013, 8, e73233. [Google Scholar] [CrossRef] [Scilit]
- Salami, D.; Capinha, C.; Sousa, C.A.; Martins, M.D.R.O.; Lord, C. Simulation models of dengue transmission in Funchal, Madeira Island: Influence of seasonality. PLoS Negl. Trop. Dis. 2020, 14, e0008679. [Google Scholar] [CrossRef] [Scilit]
- Senapati, A.; Sardar, T.; Ganguly, K.S.; Chattopadhyay, A.K.; Chattopadhyay, J. Impact of adult mosquito control on dengue prevalence in a multi-patch setting: A case study in Kolkata (2014–2015). J. Theor. Biol. 2019, 478, 139–152. [Google Scholar] [CrossRef] [Scilit]
- Tang, B.; Xiao, Y.; Tang, S.; Wu, J. Modelling weekly vector control against Dengue in the Guangdong Province of China. J. Theor. Biol. 2016, 410, 65–76. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Thomé, R.C.; Yang, H.M.; Esteva, L. Optimal control of Aedes aegypti mosquitoes by the sterile insect technique and insecticide. Math. Biosci. 2010, 223, 12–23. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wijaya, K.P.; Goetz, T.; Soewono, E. An optimal control model of mosquito reduction management in a dengue endemic region. Int. J. Biomath. 2014, 7, 1450056. [Google Scholar] [CrossRef] [Scilit]
- Winskill, P.; Harris, A.F.; A Morgan, S.; Stevenson, J.; Raduan, N.; Alphey, L.; McKemey, A.R.; A Donnelly, C. Genetic control of Aedes aegypti: Data-driven modelling to assess the effect of releasing different life stages and the potential for long-term suppression. Parasites Vectors 2014, 7, 68. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Tang, S.; Cheke, R.A. Models to assess how best to replace dengue virus vectors with Wolbachia -infected mosquito populations. Math. Biosci. 2015, 269, 164–177. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Walker, T.; Johnson, P.H.; Moreira, L.A.; Iturbe-Ormaetxe, I.; Frentiu, F.D.; McMeniman, C.J.; Leong, Y.S.; Dong, Y.; Axford, J.; Kriesner, P.; et al. The wMel Wolbachia strain blocks dengue and invades caged Aedes aegypti populations. Nature 2011, 476, 450–453. [Google Scholar] [CrossRef] [Scilit]
- Perkins, T.A.; Reiner, R.C.; Rodriguez-Barraquer, I.; Smith, D.L.; Scott, T.W.; Cummings, D.A.T. A review of transmission models of dengue: A quantitative and qualitative analysis of model features. In Dengue and Dengue Hemorrhagic Fever, 2nd ed.; CAB International: Wallingford, UK, 2014; pp. 99–114. [Google Scholar] [CrossRef] [Scilit]
- Moher, D.; Liberati, A.; Tetzlaff, J.; Altman, D.G.; PRISMA Group. Preferred reporting items for systematic reviews and meta-analyses: The PRISMA statement. PLoS Med. 2009, 6, e1000097. [Google Scholar] [CrossRef] [Scilit]
- Fone, D.L.; Hollinghurst, S.; A Temple, M.; Round, A.; Lester, N.; Weightman, A.; Roberts, K.; Coyle, E.; Bevan, G.; Palmer, S. Systematic review of the use and value of computer simulation modelling in population health and health care delivery. J. Public Health Med. 2003, 25, 325–335. [Google Scholar] [CrossRef] [Scilit]
- Harris, R.C.; Sumner, T.; Knight, G.; White, R.G. Systematic review of mathematical models exploring the epidemiological impact of future TB vaccines. Hum. Vaccines Immunother. 2016, 12, 2813–2832. [Google Scholar] [CrossRef] [Scilit]
- WHO. Dengue and Severe Dengue. 2022. Available online: https://www.who.int/news-room/fact-sheets/detail/dengue-and-severe-dengue (accessed on 15 June 2022).
- Thomas, M.B. Biological control of human disease vectors: A perspective on challenges and opportunities. Biocontrol 2018, 63, 61–69. [Google Scholar] [CrossRef] [Scilit]
- De Oliveira, S.R.; Caleffe, R.R.T.; Conte, H. Chemical control of aedes aegypti: A review on effects on the environment and human health. Revista Eletrônica Em Gestão Educ. E Tecnol. Ambiental 2017, 21, 240–247. [Google Scholar] [CrossRef] [Scilit]
- Jesus, T.; Wanner, E.; Cardoso, R. A receding horizon control approach for integrated vector management of Aedes aegypti using chemical and biological control: A mono and a multiobjective approach. Math. Methods Appl. Sci. 2019, 43, 3220–3237. [Google Scholar] [CrossRef] [Scilit]
- Lima, E.P.; Goulart, M.; Neto, M.R. Meta-analysis of studies on chemical, physical and biological agents in the control of Aedes aegypti. BMC Public Health 2015, 15, 858. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Amelia-Yap, Z.H.; Chen, C.D.; Sofian-Azirun, M.; Low, V.L. Pyrethroid resistance in the dengue vector Aedes aegypti in Southeast Asia: Present situation and prospects for management. Parasites Vectors 2018, 11, 332. [Google Scholar] [CrossRef] [Scilit]
- Fulcher, A.; Farooq, M.; Richardson, A.G.; Smith, M.L.; Scott, J.M.; Gaines, M.K.; Xue, R.-D. Characteristics and Efficacy of Three Commercial Handheld Thermal Foggers with Pyrethroid Insecticides Against Three Species of Mosquitoes. J. Am. Mosq. Control. Assoc. 2016, 32, 44–50. [Google Scholar] [CrossRef] [Scilit]
- Samuel, M.; Maoz, D.; Manrique, P.; Ward, T.; Runge-Ranzinger, S.; Toledo, J.; Boyce, R.; Horstick, O. Community effectiveness of indoor spraying as a dengue vector control method: A systematic review. PLoS Negl. Trop. Dis. 2017, 11, e0005837. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Killeen, G.F. Control of malaria vectors and management of insecticide resistance through universal coverage with next-generation insecticide-treated nets. Lancet 2020, 395, 1394–1400. [Google Scholar] [CrossRef] [Scilit]
- Okumu, F. The fabric of life: What if mosquito nets were durable and widely available but insecticide-free? Malar. J. 2020, 19, 260. [Google Scholar] [CrossRef] [Scilit]
- Manrique-Saide, P.; Che-Mendoza, A.; Barrera-Pérez, M.; Guillermo-May, G.; Herrera-Bojorquez, J.; Dzul-Manzanilla, F.; Gutiérrez-Castro, C.; Lenhart, A.; Vazquez-Prokopec, G.; Sommerfeld, J.; et al. Use of Insecticide-Treated House Screens to Reduce Infestations of Dengue Virus Vectors, Mexico. Emerg. Infect. Dis. 2015, 21, 308–311. [Google Scholar] [CrossRef] [Scilit]
- Lenhart, A.; Morrison, A.C.; Paz-Soldan, V.A.; Forshey, B.M.; Cordova-Lopez, J.J.; Astete, H.; Elder, J.P.; Sihuincha, M.; Gotlieb, E.E.; Halsey, E.S.; et al. The impact of insecticide treated curtains on dengue virus transmission: A cluster randomized trial in Iquitos, Peru. PLoS Negl. Trop. Dis. 2020, 14, e0008097. [Google Scholar] [CrossRef] [Scilit]
- Rather, I.A.; Parray, H.A.; Lone, J.B.; Paek, W.K.; Lim, J.; Bajpai, V.K.; Park, Y.-H. Prevention and Control Strategies to Counter Dengue Virus Infection. Front. Cell Infect. Microbiol. 2017, 7, 336. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- George, L.; Lenhart, A.; Toledo, J.; Lazaro, A.; Han, W.W.; Velayudhan, R.; Ranzinger, S.R.; Horstick, O. Community-Effectiveness of Temephos for Dengue Vector Control: A Systematic Literature Review. PLoS Negl. Trop. Dis. 2015, 9, e0004006. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cavany, S.M.; España, G.; Lloyd, A.L.; Waller, L.A.; Kitron, U.; Astete, H.; Elson, W.H.; Vazquez-Prokopec, G.M.; Scott, T.W.; Morrison, A.C.; et al. Optimizing the deployment of ultra-low volume and targeted indoor residual spraying for dengue outbreak response. PLoS Comput. Biol. 2020, 16, e1007743. [Google Scholar] [CrossRef] [Scilit]
- Paiva, C.N.; Lima, J.W.D.O.; Camelo, S.S.; Lima, C.D.F.; Cavalcanti, L.P.D.G. Survival of larvivorous fish used for biological control of Aedes aegypti (Diptera: Culicidae) combined with different larvicides. Trop. Med. Int. Health 2014, 19, 1082–1086. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Han, W.W.; Lazaro, A.; McCall, P.; George, L.; Runge-Ranzinger, S.; Toledo, J.; Velayudhan, R.; Horstick, O. Efficacy and community effectiveness of larvivorous fish for dengue vector control. Trop. Med. Int. Health 2015, 20, 1239–1256. [Google Scholar] [CrossRef] [Scilit]
- Morales-Pérez, A.; Nava-Aguilera, E.; Legorreta-Soberanis, J.; Cortés-Guzmán, A.J.; Balanzar-Martínez, A.; Harris, E.; Coloma, J.; Alvarado-Castro, V.M.; Bonilla-Leon, M.V.; Morales-Nava, L.; et al. “Where we put little fish in the water there are no mosquitoes:” A cross-sectional study on biological control of the Aedes aegypti vector in 90 coastal-region communities of Guerrero, Mexico. BMC Public Health 2017, 17, 433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Lazaro, A.; Han, W.W.; George, L.; Velayudhan, R.; Toledo, J.; Ranzinger, S.R.; Horstick, O.; Manrique-Saide, P. Community effectiveness of copepods for dengue vector control: Systematic review. Trop. Med. Int. Health 2015, 20, 685–706. [Google Scholar] [CrossRef] [Scilit]
- Udayanga, N.L.; Ranathunge, T.; Iqbal, M.C.M.; Abeyewickreme, W.; Hapugoda, M. Predatory efficacy of five locally available copepods on Aedes larvae under laboratory settings: An approach towards bio-control of dengue in Sri Lanka. PLoS ONE 2019, 14, e0216140. [Google Scholar] [CrossRef] [Scilit]
- Bohari, R.; Hin, C.J.; Matusop, A.; Abdullah, M.R.; Ney, T.G.; Benjamin, S.; Lim, L.H. Wide area spray of bacterial larvicide, Bacillus thuringiensis israelensis strain AM65-52, integrated in the national vector control program impacts dengue transmission in an urban township in Sibu district, Sarawak, Malaysia. PLoS ONE 2020, 15, e0230910. [Google Scholar] [CrossRef] [Scilit]
- Boyce, R.; Lenhart, A.; Kroeger, A.; Velayudhan, R.; Roberts, B.; Horstick, O. Bacillus thuringiensis israelensis (Bti) for the control of dengue vectors: Systematic literature review. Trop. Med. Int. Health 2013, 18, 564–577. [Google Scholar] [CrossRef] [Scilit]
- Carvalho, K.D.; Crespo, M.M.; Araujo, A.P.; da Silva, R.S.; de Melo-Santos, M.A.V.; de Oliveira, C.M.F.; Silva-Filha, M.H.N.L. Long-term exposure of Aedes aegypti to Bacillus thuringiensis svar. israelensis did not involve altered susceptibility to this microbial larvicide or to other control agents. Parasites Vectors 2018, 11, 673. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kittayapong, P.; Ninphanomchai, S.; Limohpasmanee, W.; Chansang, C.; Chansang, U.; Mongkalangoon, P. Combined sterile insect technique and incompatible insect technique: The first proof-of-concept to suppress Aedes aegypti vector populations in semi-rural settings in Thailand. PLoS Negl. Trop. Dis. 2019, 13, e0007771. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zheng, X.; Zhang, D.; Li, Y.; Yang, C.; Wu, Y.; Liang, X.; Liang, Y.; Pan, X.; Hu, L.; Sun, Q.; et al. Incompatible and sterile insect techniques combined eliminate mosquitoes. Nature 2019, 572, 56–61. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qsim, M.; Ashfaq, U.A.; Yousaf, M.Z.; Masoud, M.; Rasul, I.; Noor, N.; Hussain, A. Genetically Modified Aedes aegypti to Control Dengue: A Review. Crit. Rev. Eukaryot. Gene Expr. 2017, 27, 331–340. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Olson, K.E.; Franz, A.W. Advances in genetically modified Aedes aegypti to control transmission of dengue viruses. Futur. Virol. 2015, 10, 609–624. [Google Scholar] [CrossRef] [Scilit]
- Golstein, C.; Boireau, P.; Pagès, J.-C. Benefits and limitations of emerging techniques for mosquito vector control. Comptes Rendus Biol. 2019, 342, 270–272. [Google Scholar] [CrossRef] [Scilit]
- Joubert, D.A.; Walker, T.; Carrington, L.B.; De Bruyne, J.T.; Kien, D.H.T.; Hoang, N.L.T.; Chau, N.V.V.; Iturbe-Ormaetxe, I.; Simmons, C.P.; O’Neill, S.L. Establishment of a Wolbachia Superinfection in Aedes aegypti Mosquitoes as a Potential Approach for Future Resistance Management. PLoS Pathog. 2016, 12, e1005434. [Google Scholar] [CrossRef] [Scilit]
- Jr, R.C.R.; Achee, N.; Barrera, R.; Burkot, T.R.; Chadee, D.D.; Devine, G.; Endy, T.; Gubler, D.; Hombach, J.; Kleinschmidt, I.; et al. Quantifying the Epidemiological Impact of Vector Control on Dengue. PLoS Negl. Trop. Dis. 2016, 10, e0004588. [Google Scholar] [CrossRef] [Scilit]
- Ndii, M.Z.; Hickson, R.; Allingham, D.; Mercer, G. Modelling the transmission dynamics of dengue in the presence of Wolbachia. Math. Biosci. 2015, 262, 157–166. [Google Scholar] [CrossRef] [Scilit]
- Carvalho, S.A.; da Silva, S.O.; Charret, I.D.C. Mathematical modeling of dengue epidemic: Control methods and vaccination strategies. Theory Biosci. 2019, 138, 223–239. [Google Scholar] [CrossRef] [Scilit]
- Perera, S.; Perera, S.S.N. Mathematical modeling and analysis of innate and humoral immune responses to dengue infections. Int. J. Biomath. 2019, 12, 1950077. [Google Scholar] [CrossRef] [Scilit]
- Zhao, S.; Musa, S.S.; Meng, J.; Qin, J.; He, D. The long-term changing dynamics of dengue infectivity in Guangdong, China, from 2008-2018: A modelling analysis. Trans. R. Soc. Trop. Med. Hyg. 2020, 114, 62–71. [Google Scholar] [CrossRef] [Scilit] [PubMed]
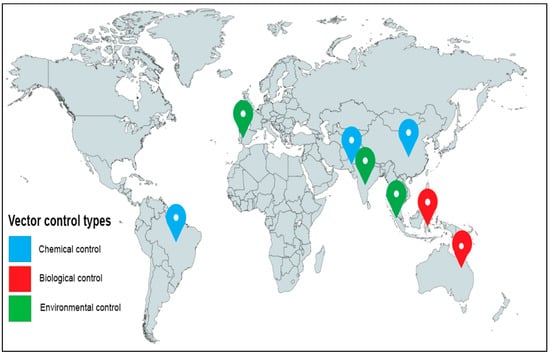

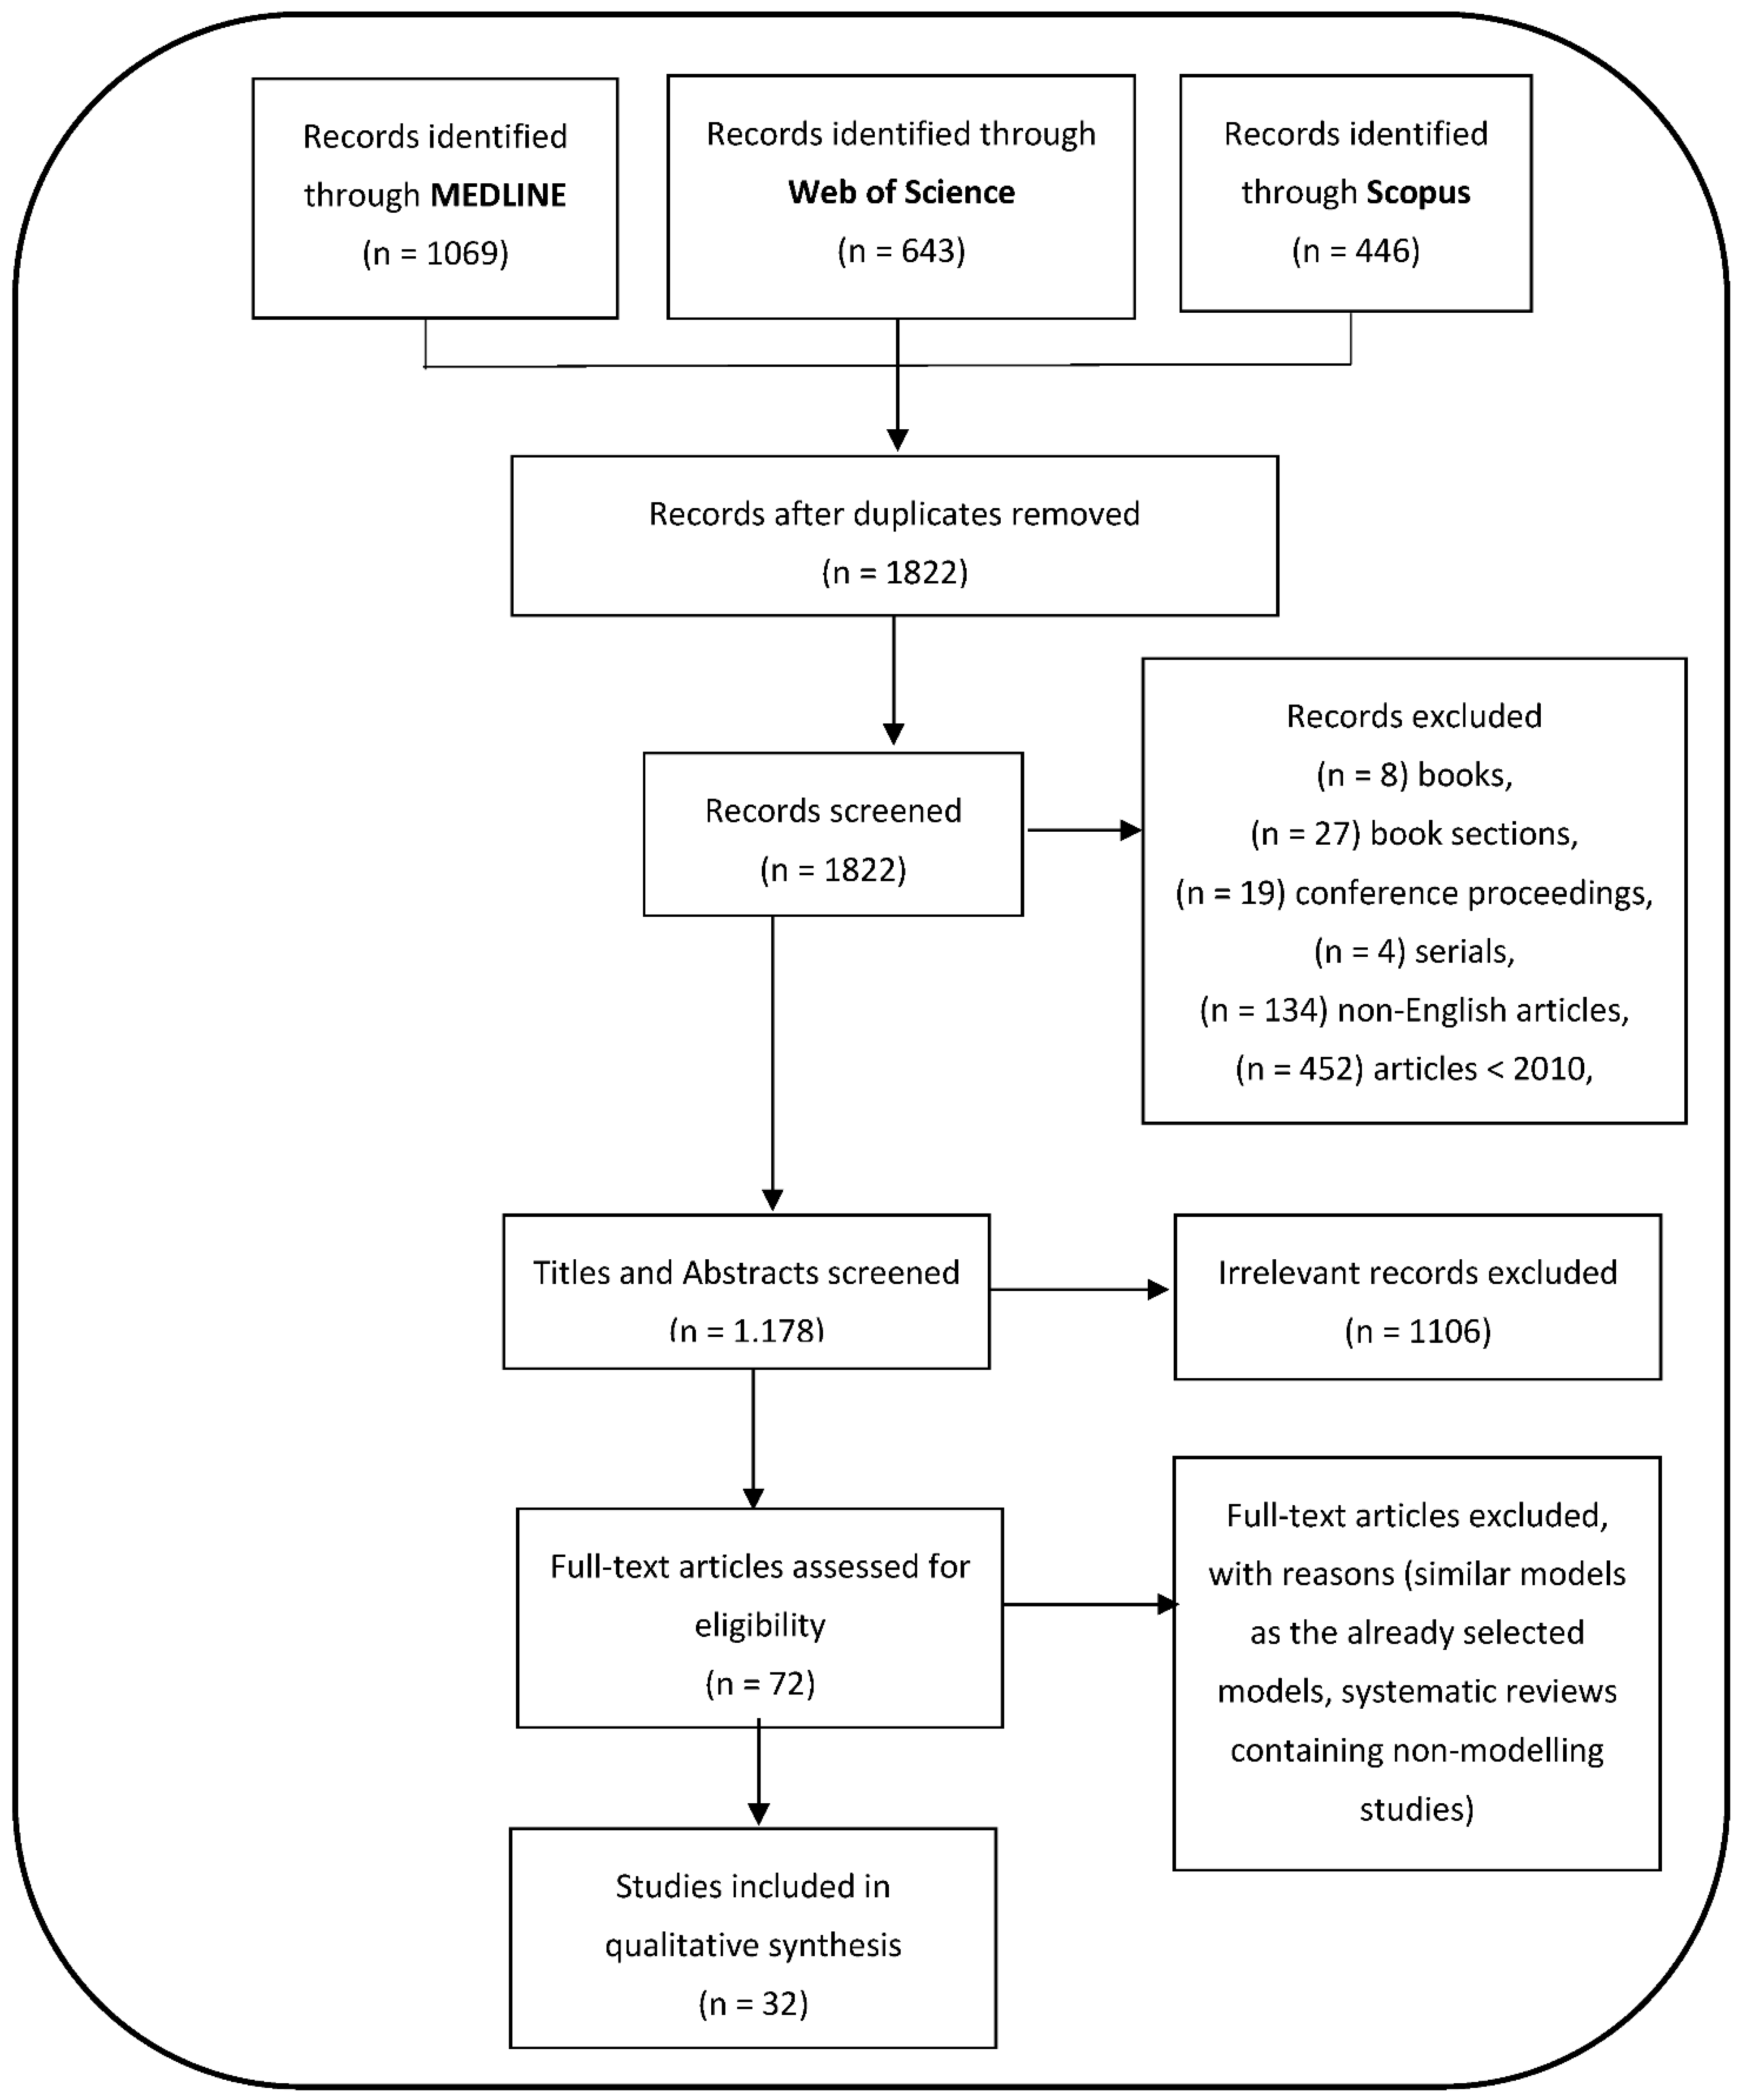
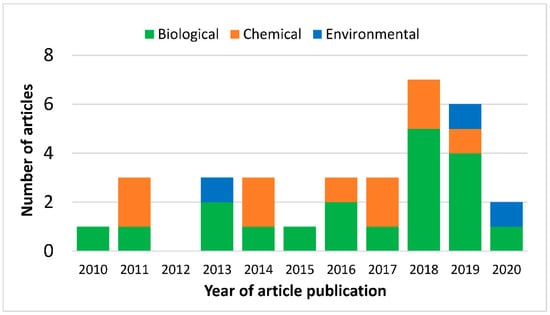
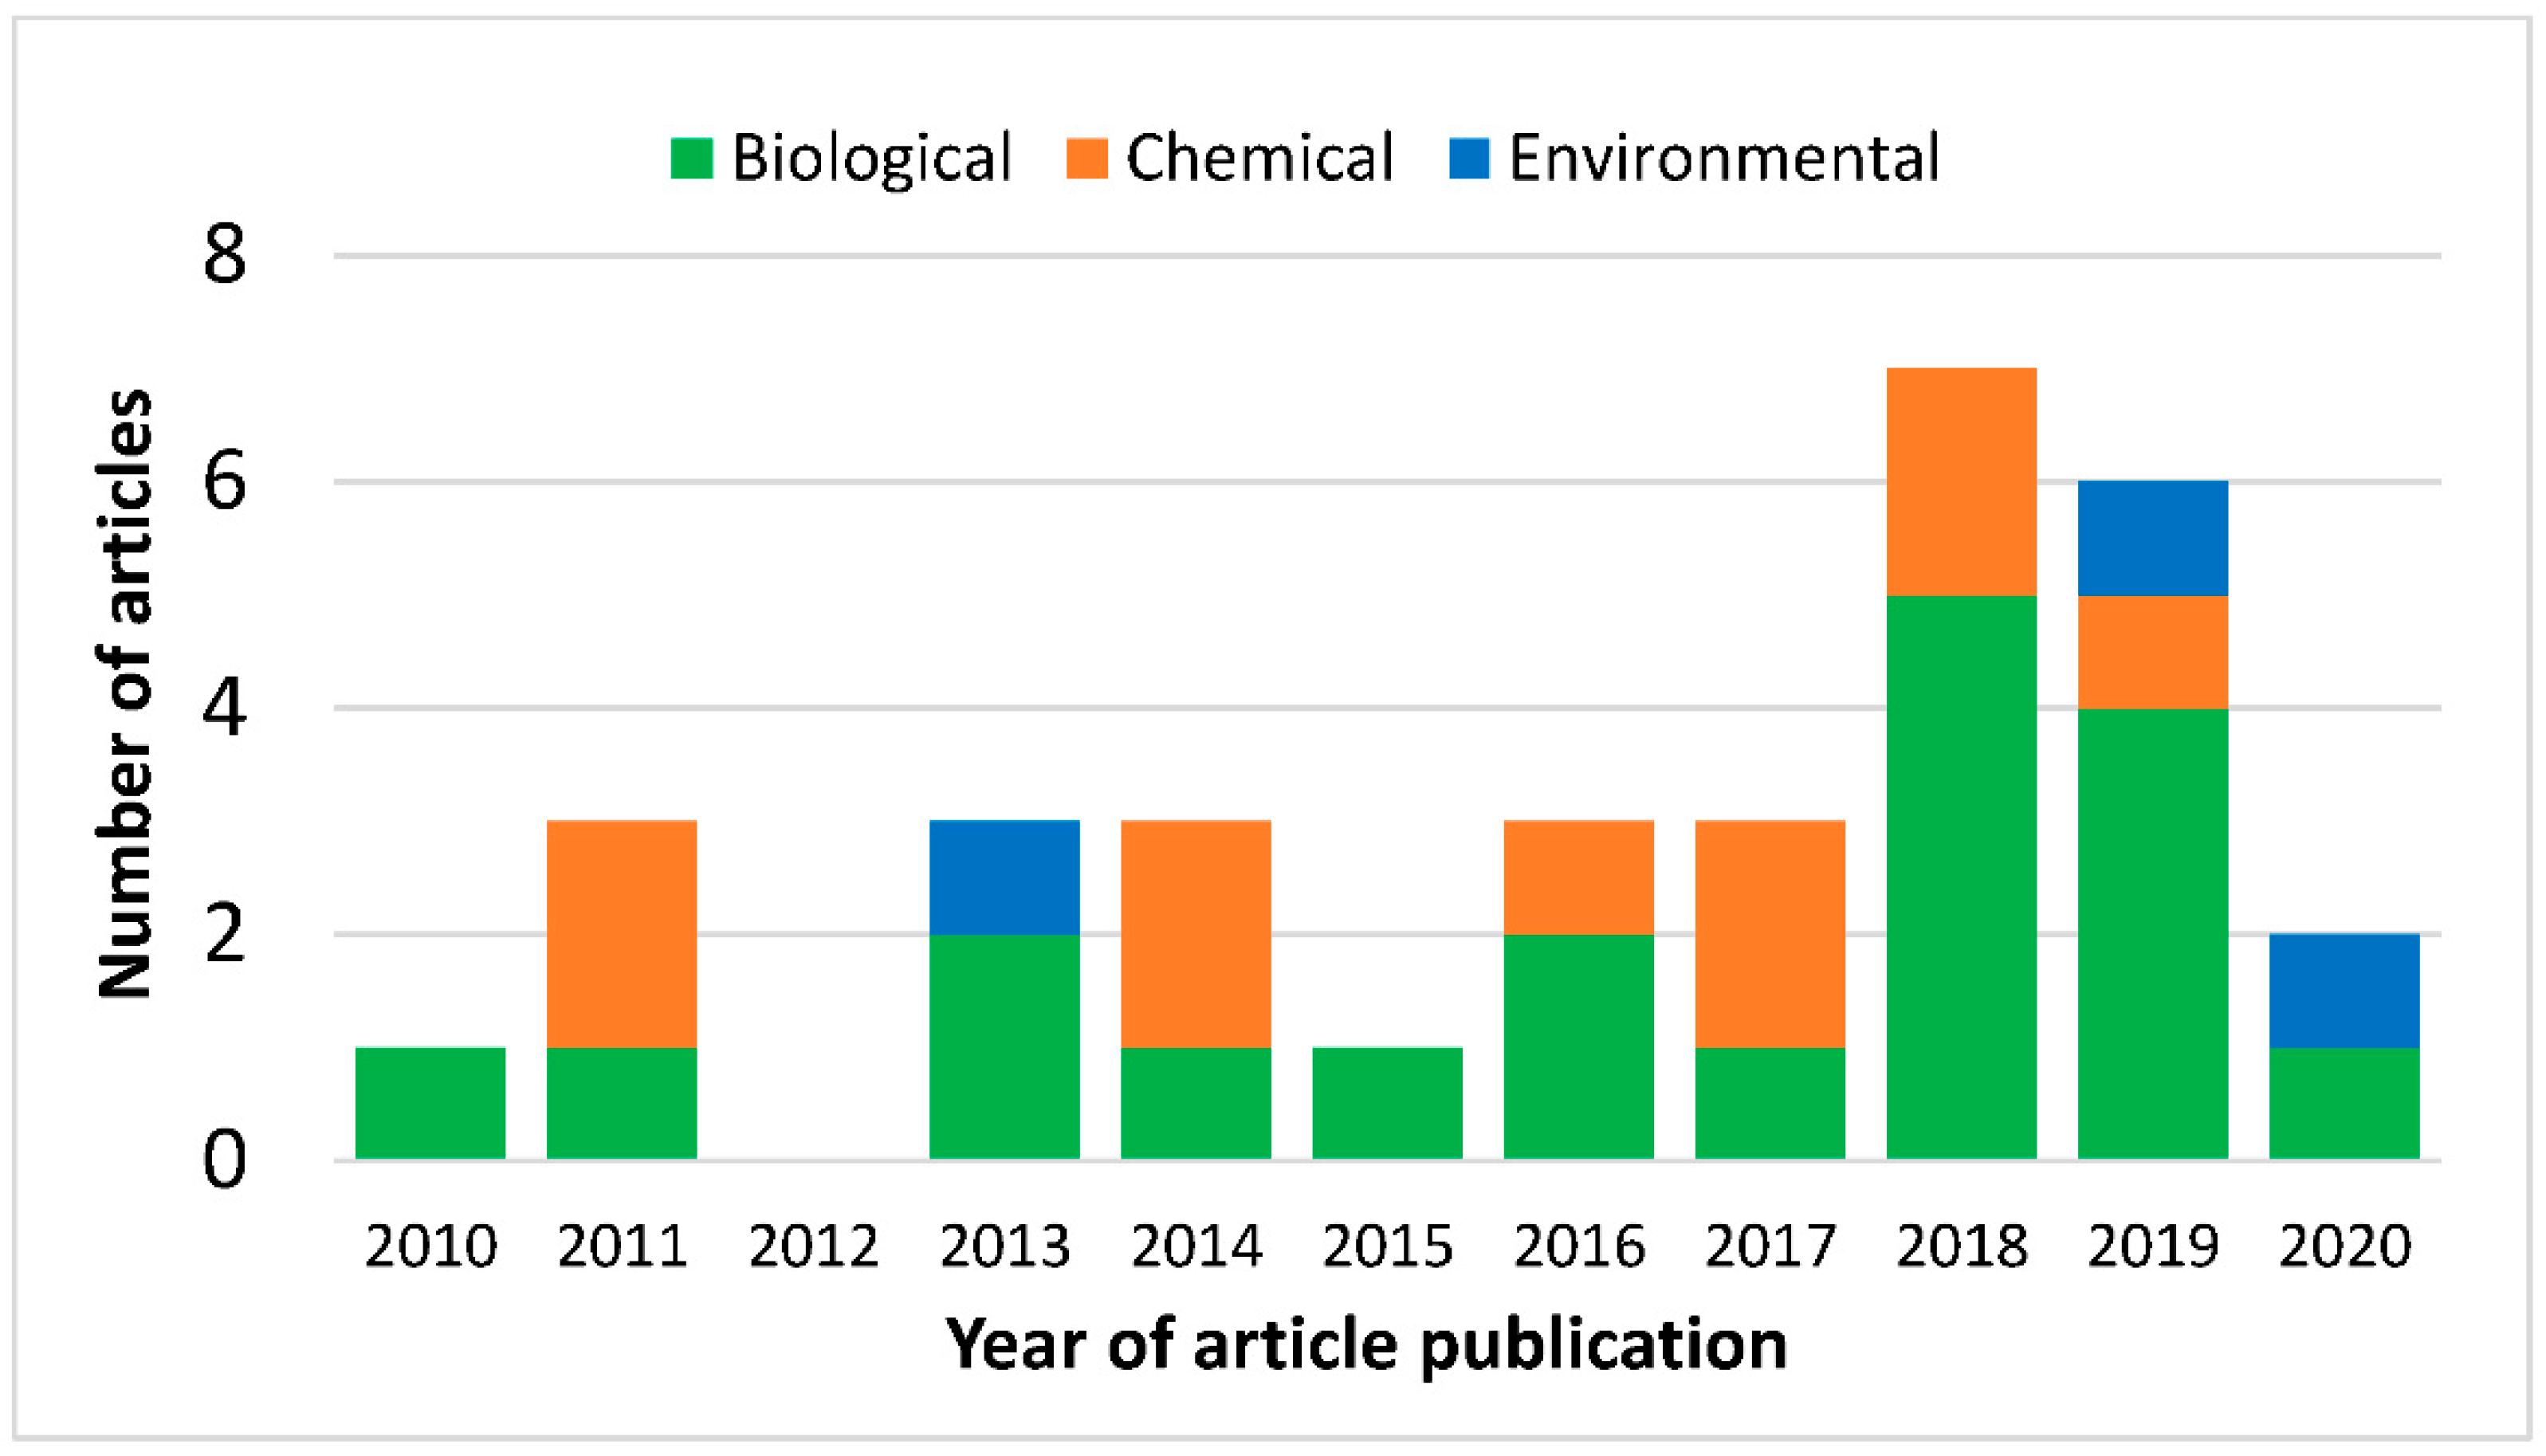
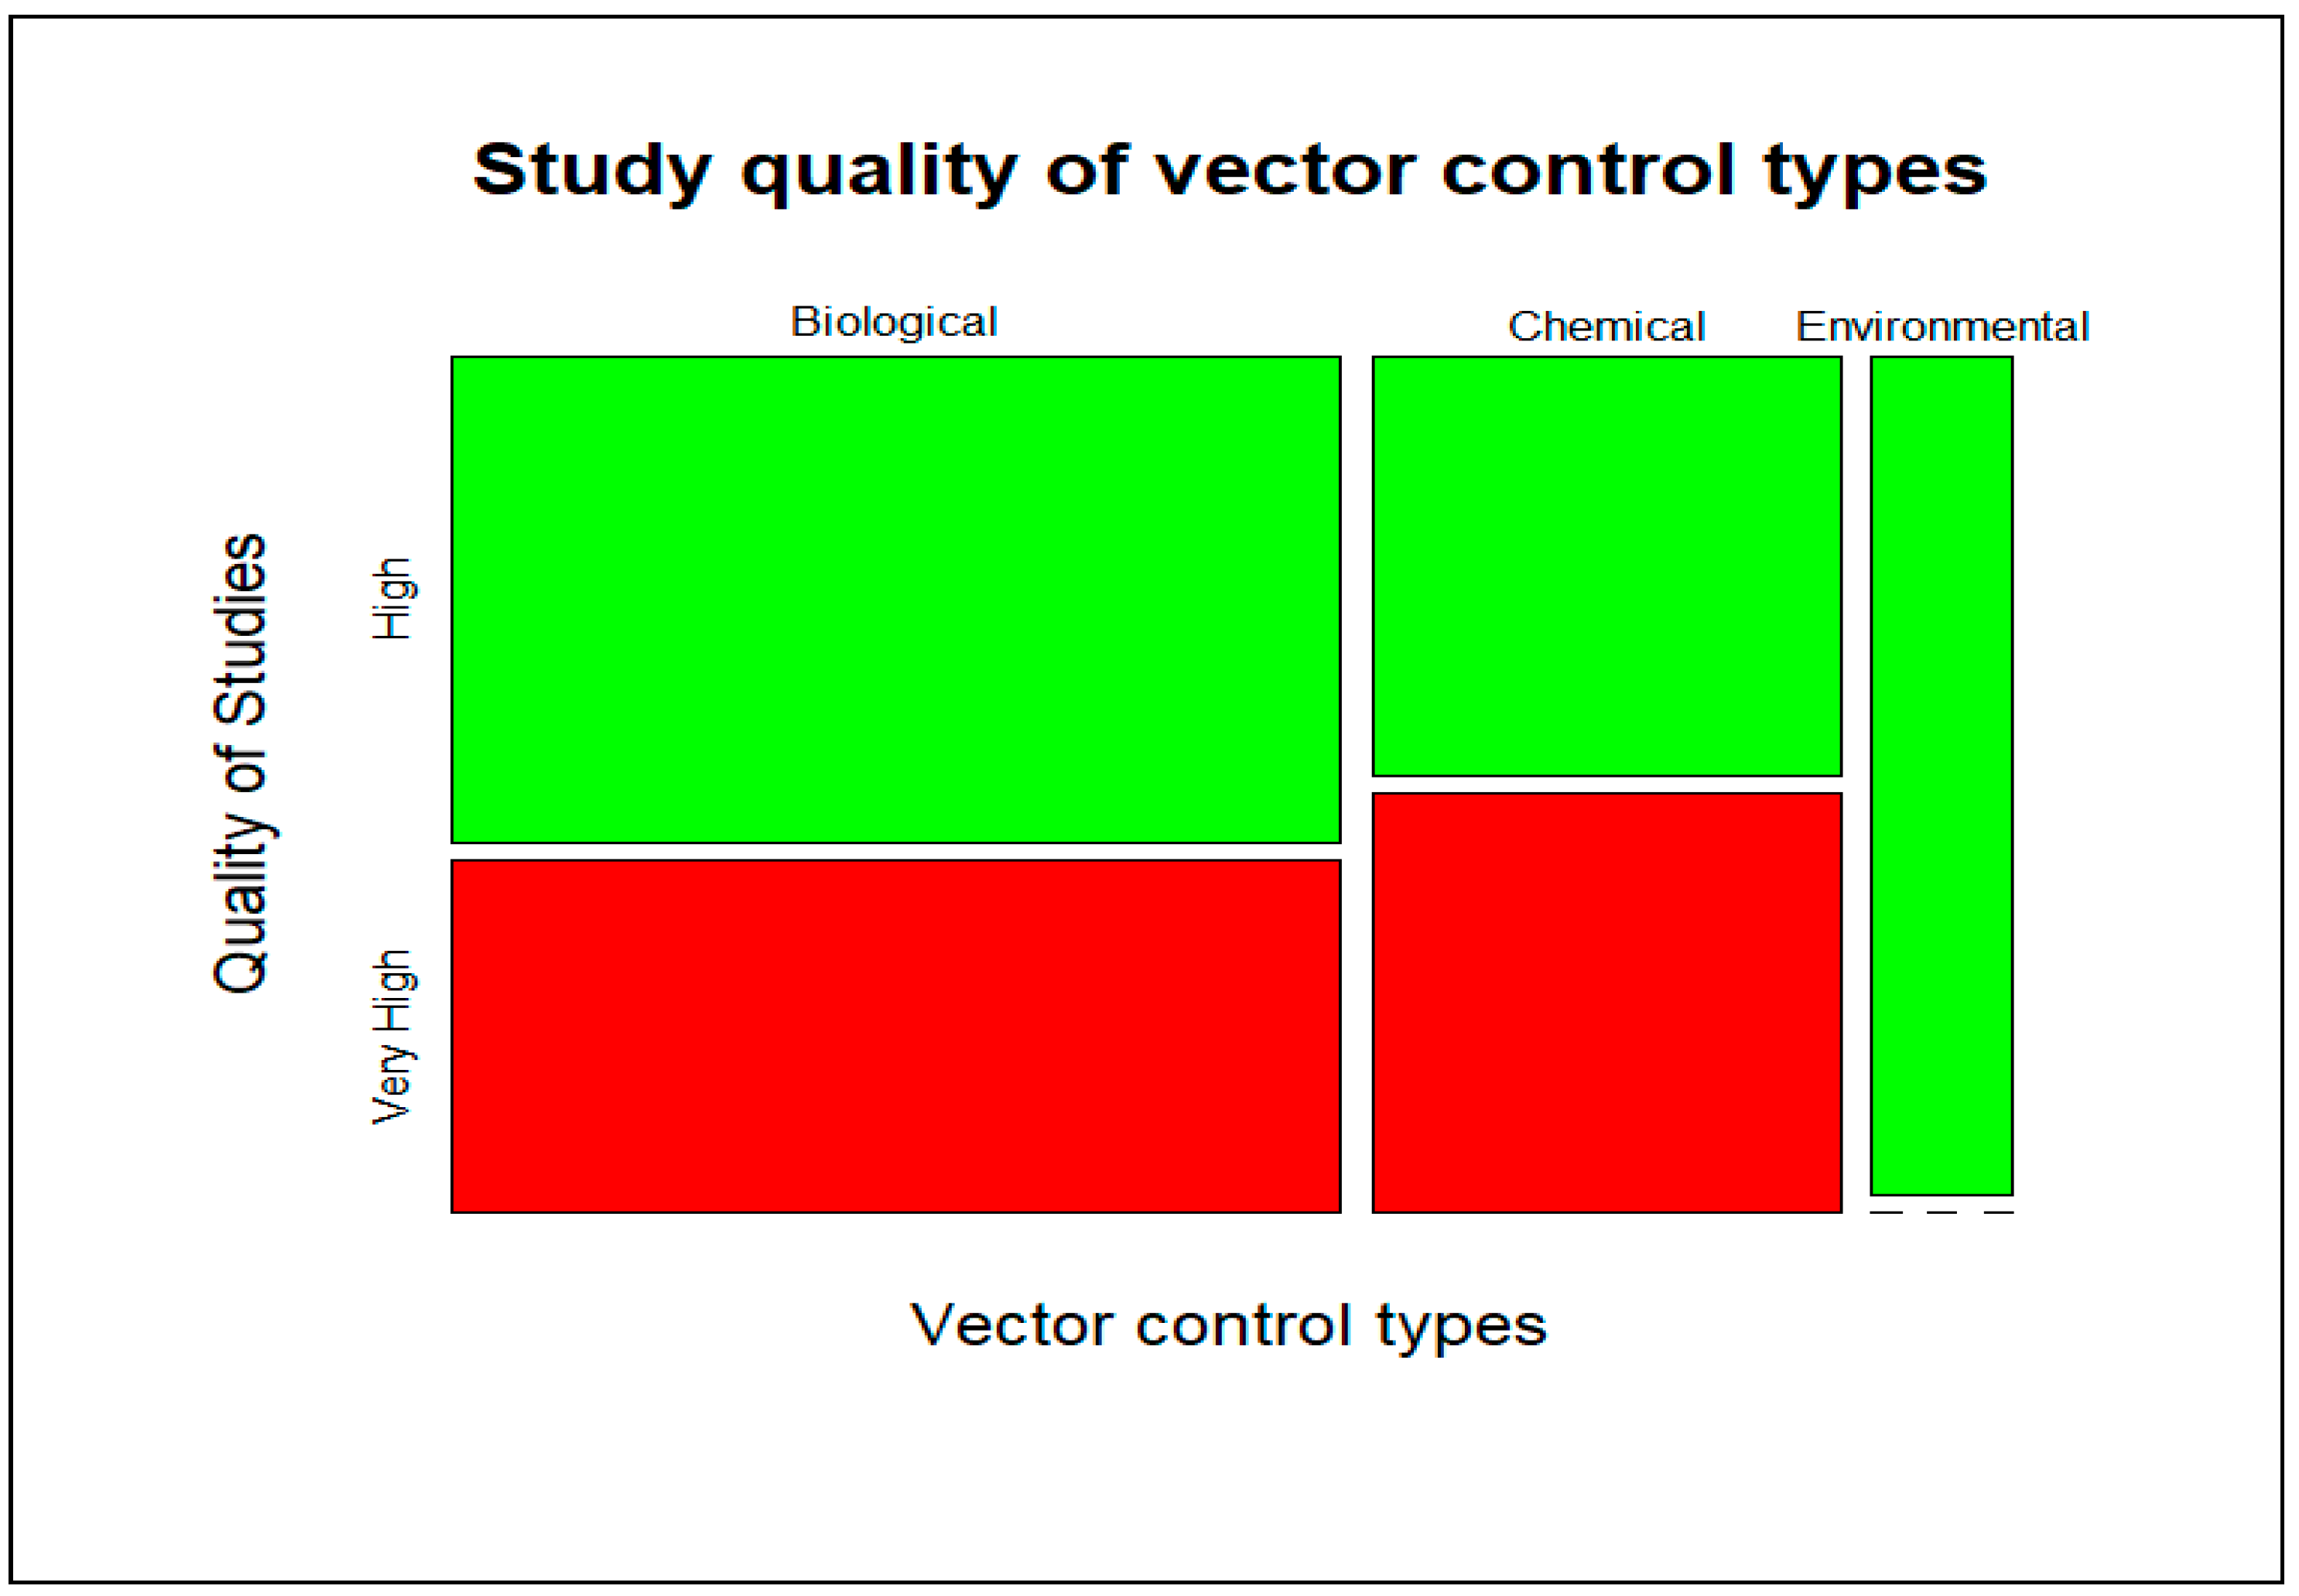

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2023 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).