


Abstract
Tropaeolum tuberosum Ruíz and Pav. “Mashua” is a crop from the Andean region associated with preventing chronic degenerative diseases. This study evaluated the content of bioactive compounds (phenolics, glucosinolates, carotenoids, and ascorbic acid) in twenty-seven Peruvian mashua morphotypes. Furthermore, three morphotypes (MAC 067, MAC 092, and MAC 123) were selected to evaluate further the effect of methyl jasmonate (MeJA) on the accumulation of bioactive compounds. Phenolic content in the mashua morphotypes ranged from 2990.76 ± 273.5 mg/kg to 24,217.36 ± 1144 mg/kg; whereas carotenoids ranged from 12.8 ± 0.6 mg/kg to 85.8 ± 3.1 mg/kg. Moreover, total glucosinolate content ranged from 65 ± 11 mmol/kg to 1289 ± 65 mmol/kg. The different mashua morphotypes showed low levels of ascorbic acid (lower than 5 mg/kg) compared with other crops. Except for glucosinolates, MeJA application augmented the level of bioactive compounds, showing increases of up to 150.1%, 535.0%, and 542% for total phenolics, carotenoids, and ascorbic acid, respectively. Results indicated that mashua is an excellent source of phenolics and glucosinolates, whereas it contains adequate levels of carotenoids and low levels of vitamin C. MeJA application during postharvest represented a simple approach to increase the content of bioactive compounds in mashua.
1. Introduction
Tropaeolum tuberosum Ruíz and Pav. “Mashua” is a relevant crop of the Andean region, whose origin seems to be the center of the Andes [1]. Perú has a high diversity of mashua, accounting for more than 200 morphotypes. Mashua is an herbaceous plant native to the central Andes. It is generally cultivated with other tubers between 2400 and 4300 altitudes [2,3]. Moreover, mashua is the fourth crop of economic importance in the Andean region after potato, oca, and olluco [4,5]. The main variations in the content of bioactive compounds in mashua morphotypes are attributed to the differences in genetic biodiversity [1,2].
From an agronomic viewpoint, mashua is a native plant cultivated in poor soils where agroclimatic conditions are adverse, the use of fertilizers and pesticides is not required, and despite these conditions in which it grows, the production yield exceeds other tubers, such as potatoes. In addition, it is a frost-tolerant crop that is planted in Bolivia, Perú, Ecuador, Colombia, Venezuela, and Argentina [4].
Mashua is barely known in the local and international markets. However, polar extracts and isolated compounds from the tuber have demonstrated numerous in vitro and in vivo pharmacological activities, including antioxidant, diuretic, anti-inflammatory, and anticancer properties, due to the bioactive compounds present in the plant [6,7]. Phytochemicals found in mashua include glucosinolates, hydroxybenzoic acids, flavanols, tannis, anthocyanins, isothiocyanates, alkamides, phytosterols, and fatty acids [7]. All these phytochemicals have been related to the prevention and treatment of chronic and generative diseases.
The use of controlled postharvest abiotic stresses, such as applying exogenous phytohormones such as methyl jasmonate (MeJA), has been shown to increase the content of secondary metabolites in plants [8,9]. For instance, its application in plant tissues increases the concentration of phenolic compounds in carrots [10] and glucosinolates in broccoli heads [11].
The objective of the present study was to evaluate the content of total phenolics, glucosinolates, carotenoids, and ascorbic acid in twenty-seven Peruvian mashua morphotypes and determine the effect of postharvest MeJA application on the accumulation of secondary metabolites in the tuber.
2. Materials and Methods
2.1. Chemicals
Sulfatase from Helix pomatia, sinigrin hydrate, Sephadex A-25, methanol (HPLC grade), sodium acetate, MeJA, ascorbic acid, N-ethylmaleimide (NEM), dichloro-diphenyl-trichloroethane (DDT), α,α′-bipyridyl, and orthophosphoric acid were obtained from Sigma Chemical Co. (St. Louis, MO, USA). Desulfoglucoraphanin was obtained from Santa Cruz Biotechnology (Dallas, TX, USA). All other chemicals (ethanol, acetone, FeCl3, H3PO4, trichloroacetic acid (TCA), and liquid nitrogen) were purchased from Desarrollo de Especialidades Químicas S.A. de C.V. (San Nicolás de los Garza, NL, México).
2.2. Plant Material and Methyl Jasmonate (MeJA) Treatments
The twenty-seven morphotypes of mashua were harvested in Perú in the locations indicated in Table 1. The color of the tubers analyzed included yellow, black, and white (Table 1). Except for mashua morphotypes subjected to MeJA treatments, the samples were frozen with liquid nitrogen, ground to a fine powder, freeze-dried, and stored at −80 °C until further analysis.
Table 1.
Harvest location and tuber color of twenty-seven Peruvian mashua morphotypes.
The effect of MeJA on the accumulation of bioactive compounds in mashua was evaluated in three morphotypes (MAC 067, MAC 092, and MAC 123). MeJA was applied over a Petri dish (0.25 mL per L) by wetting a Whatman No. 4 filter paper (Whatman Inc., Piscataway, NJ, USA) to obtain a concentration of 250 ppm in the headspace, as previously described by Villarreal-García et al. [11]. The samples were stored in hermetically closed 1 L plastic containers and ventilated every 12 h to avoid CO2 accumulation in the headspace. Samples were stored for 3 days at 20 °C. The filter paper containing MeJA was replaced every 12 h at the ventilation time. The control was stored under the same conditions without applying MeJA. After MeJA treatment, samples were frozen with liquid nitrogen, ground to a fine powder, freeze-dried, and stored at −80 °C until further analysis.
2.3. Phytochemical Analyses
2.3.1. Extraction and Quantification of Total Free Phenolics
For the extraction of free phenolic compounds, freeze-dried mashua samples (0.5 g dry weight) were mixed with methanol (20 mL) and ultrasonicated in an ultrasound bath (Branson 2510, Branson Ultrasonic Corporation, Danbury, CT, USA) for 5 min. Centrifugation was performed at 13,000× g for 5 min at 4 °C. Total phenolics were determined by the Folin–Ciocalteu method adapted to a 96-well microplate format [12,13]. Chlorogenic acid was used as standard, and the total phenolic content was expressed as mg of chlorogenic acid equivalents per kg of mashua dry weight (DW).
2.3.2. Extraction and Quantification of Total Glucosinolates
The extraction of glucosinolates was performed as reported by Villarreal-García et al. [11]. Briefly, methanol/water (10 mL, 70:30 v:v, 70 °C) was added to mashua powder (0.2 g). Then, sinigrin hydrate was incorporated as an internal standard (50 µL, 3 mM) and incubated (70 °C for 30 min) to inactivate myrosinase. Extracts were left to cool at room temperature and centrifuged (18,000× g, 10 min, 4 °C). After extraction, the glucosinolates were desulfated and purified as described by Villareal-García et al. [11].
Desulfoglucosinolates were identified and quantified using a high-performance liquid chromatography system comprised of a quaternary pump, an autosampler, and a diode array detector (1260 Infinity, Agilent Technologies, Santa Clara, CA, USA). The column separating desulfoglucosinolates was a 4.6 mm × 250 mm, 5 μm, C18 reverse-phase column (Luna, Phenomenex, Torrace, CA, USA). Chromatographic conditions were as described by Villarreal-García et al. [11]. Desulfoglucosinolates were detected at 227 nm. The areas under the curve of chromatographic picks corresponding to desulfoglucosinolates were added to determine the total glucosinolate content. To quantify glucosinolates, a standard curve of desulfoglucoraphanin was prepared in the range of 0–700 μM. The concentration of total glucosinolates was expressed as mmol of desulfoglucoraphanin equivalents per kg of mashua DW.
2.3.3. Extraction and Quantification of Total Carotenoids
Total carotenoids were extracted following the procedure described by Cuéllar-Villarreal et al. [14]. Freeze-dried mashua powder (0.2 g) was homogenized with a solution (15 mL) containing acetone/ethanol (1:1) with 200 mg/L BHT added. The homogenates were vacuum filtered through Whatmann No. 1 filter paper (Piscataway, NJ, USA), and the acetone/ethanol extract was recovered. This procedure was repeated 4 times to ensure complete extraction of carotenoids in the samples. The obtained acetone/ethanol extracts were combined before quantification of carotenoids. The absorbance of the acetone/ethanol extracts was measured at 470 nm using a Genesys 10S UV–vis Spectrophotometer (Thermo Scientific, Waltham, MA, USA). Total carotenoids were calculated with Equation (1) [15]:
where TC refers to total carotenoids, V is the extract volume, A is the absorbance, A1% is the extinction coefficient for a mixture of solvents arbitrarily set at 2500, and G is the sample weight in g. Total carotenoids were reported as mg per kg of mashua DW.
2.3.4. Extraction and Quantification of Ascorbic Acid
Ascorbic acid was quantified with the method of Gillespie and Ainsworth [16]. A freeze-dried mashua sample (50 mg) was homogenized with trichloroacetic acid (TCA, 6%, 5 mL). The extract (100 μL) was added to the DDT solution (32 mM, 50 μL) and incubated for 10 min. After that, NEM (12 mM, 50 μL) was added and incubated for 30 s. Then, a mixture of α,α′-bipyridyl (4%, 200 μL), FeCl3 (3%, 100 μL), H3PO4 (43%, 200 μL), and TCA (10%, 250 μL) and incubated at 37 °C for 60 min. Finally, the absorbance of the reactions was recorded at 525 nm. Absorbance values were compared against an ascorbic acid standard curve (0.10–3 mM) prepared in TCA (6%). Results were expressed as mg of ascorbic acid per kg of mashua DW.
2.4. Statistical Analysis
All reported data were obtained from repeated independent extractions and quantifications. There were three biological repetitions for evaluating phytochemicals per morphotype (n = 3). The data represent the mean values of samples and their standard error. Analyses of variance (ANOVA) were conducted using JMP software version 16.0 (SAS Institute Inc., Cary, NC, USA), and mean separations were achieved with the LSD test (p < 0.05).
3. Results and Discussion
3.1. Phytochemical Characterization of Peruvian Mashua Morphotypes
Phenolic compounds are related to the prevention of different diseases, mainly due to the direct antioxidant activity against free radicals [17]. The content of total phenolics in the different mashua cultivars ranged from 2990.76 ± 273.5 mg/kg (MAC 090) to 24,217.36 ± 1144 mg/kg (MAC 092) (Table 2). These results are in the range of phenolic compounds content previously reported for ARB 5241 and DP 0224 mashua morphotypes [18]. Moreover, the total phenolics quantified match the color of the mashua morphotypes. For instance, MAC 090 is white, whereas MAC 092 is black (Table 1), indicating that MAC 092 has a higher level of phenolics, mainly anthocyanins [18]. Compared with other vegetables, mashua morphotype MAC 092 is around the total phenolic content of sweet cherry (20,980 mg/kg) and 210% higher than purple potato, which is another tuber with high levels of phenolics [19].
Table 2.
Total phenolics, carotenoids, glucosinolates, and ascorbic acid content of twenty-seven Peruvian mashua morphotypes.
Carotenoids are pigments responsible for the yellow–orange–red color of plant tissues. Carotenoids also possess high antioxidant activity, mainly due to their singlet oxygen and free radical reactions [21]. Regarding the total carotenoids, the content in the different morphotypes evaluated ranged from 12.8 ± 0.6 mg/kg (MAC 095) to 85.8 ± 3.1 mg/kg (MAC 069). These results do not match the mashua tuber’s color, where MAC 095 has a grayish-purple color and the MAC 069 is brown, indicating that darker colors cover the yellow–orange–red color of carotenoids present in mashua.
Glucosinolates are sulfur and nitrogen-containing thioglucosides derived from glucose and amino acids. They are mainly found in the Brassicaceae family [22,23]. The total glucosinolate content ranged from 65 ± 11 mmol/kg (MAC 135) to 1289 ± 65 mmol/kg (MAC 123). Compared with broccoli sprouts, one of the food sources with the highest content of glucosinolates, MAC 136, is in the range of previously reported values (56 ± 5 mmol/kg), whereas MAC 123 contains 2200% higher content [24]. These results indicate that mashua is an excellent source of glucosinolates.
Regarding ascorbic acid content, the values quantified in the different mashua morphotypes ranged from 0.65 ± 0.33 mg/kg (MAC 095) to 4.51 ± 0.33 mg/kg (MAC 098), which is low content compared with other sources rich in vitamin C such as strawberry (1000 mg/kg) [25]. A correlation analysis revelated that except for the color, the other factors that varied between the morphotypes (i.e., location, altitude, etc.) did not affect the content of bioactive compounds. In this context, the data showed that the darker the color of a morphotype, the higher the content of phenolics quantified (R2 = 0.7).
3.2. Effect of Methyl Jasmonate (MeJA) on the Accumulation of Bioactive Compounds of Peruvian Mashua Morphotypes
MeJA is a phytohormone that has been identified as a vital cellular regulator that mediates diverse developmental processes and plants’ defense responses against biotic and abiotic stresses. For instance, MeJA is responsible for the perception and transduction of wound signals through the octadecanoid pathway [10,26].
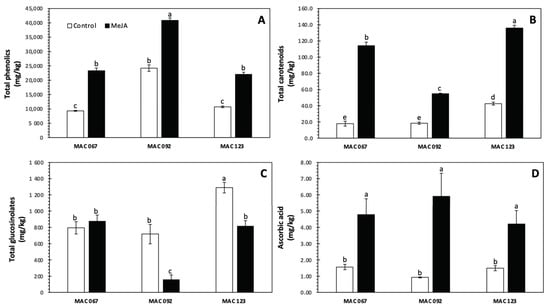
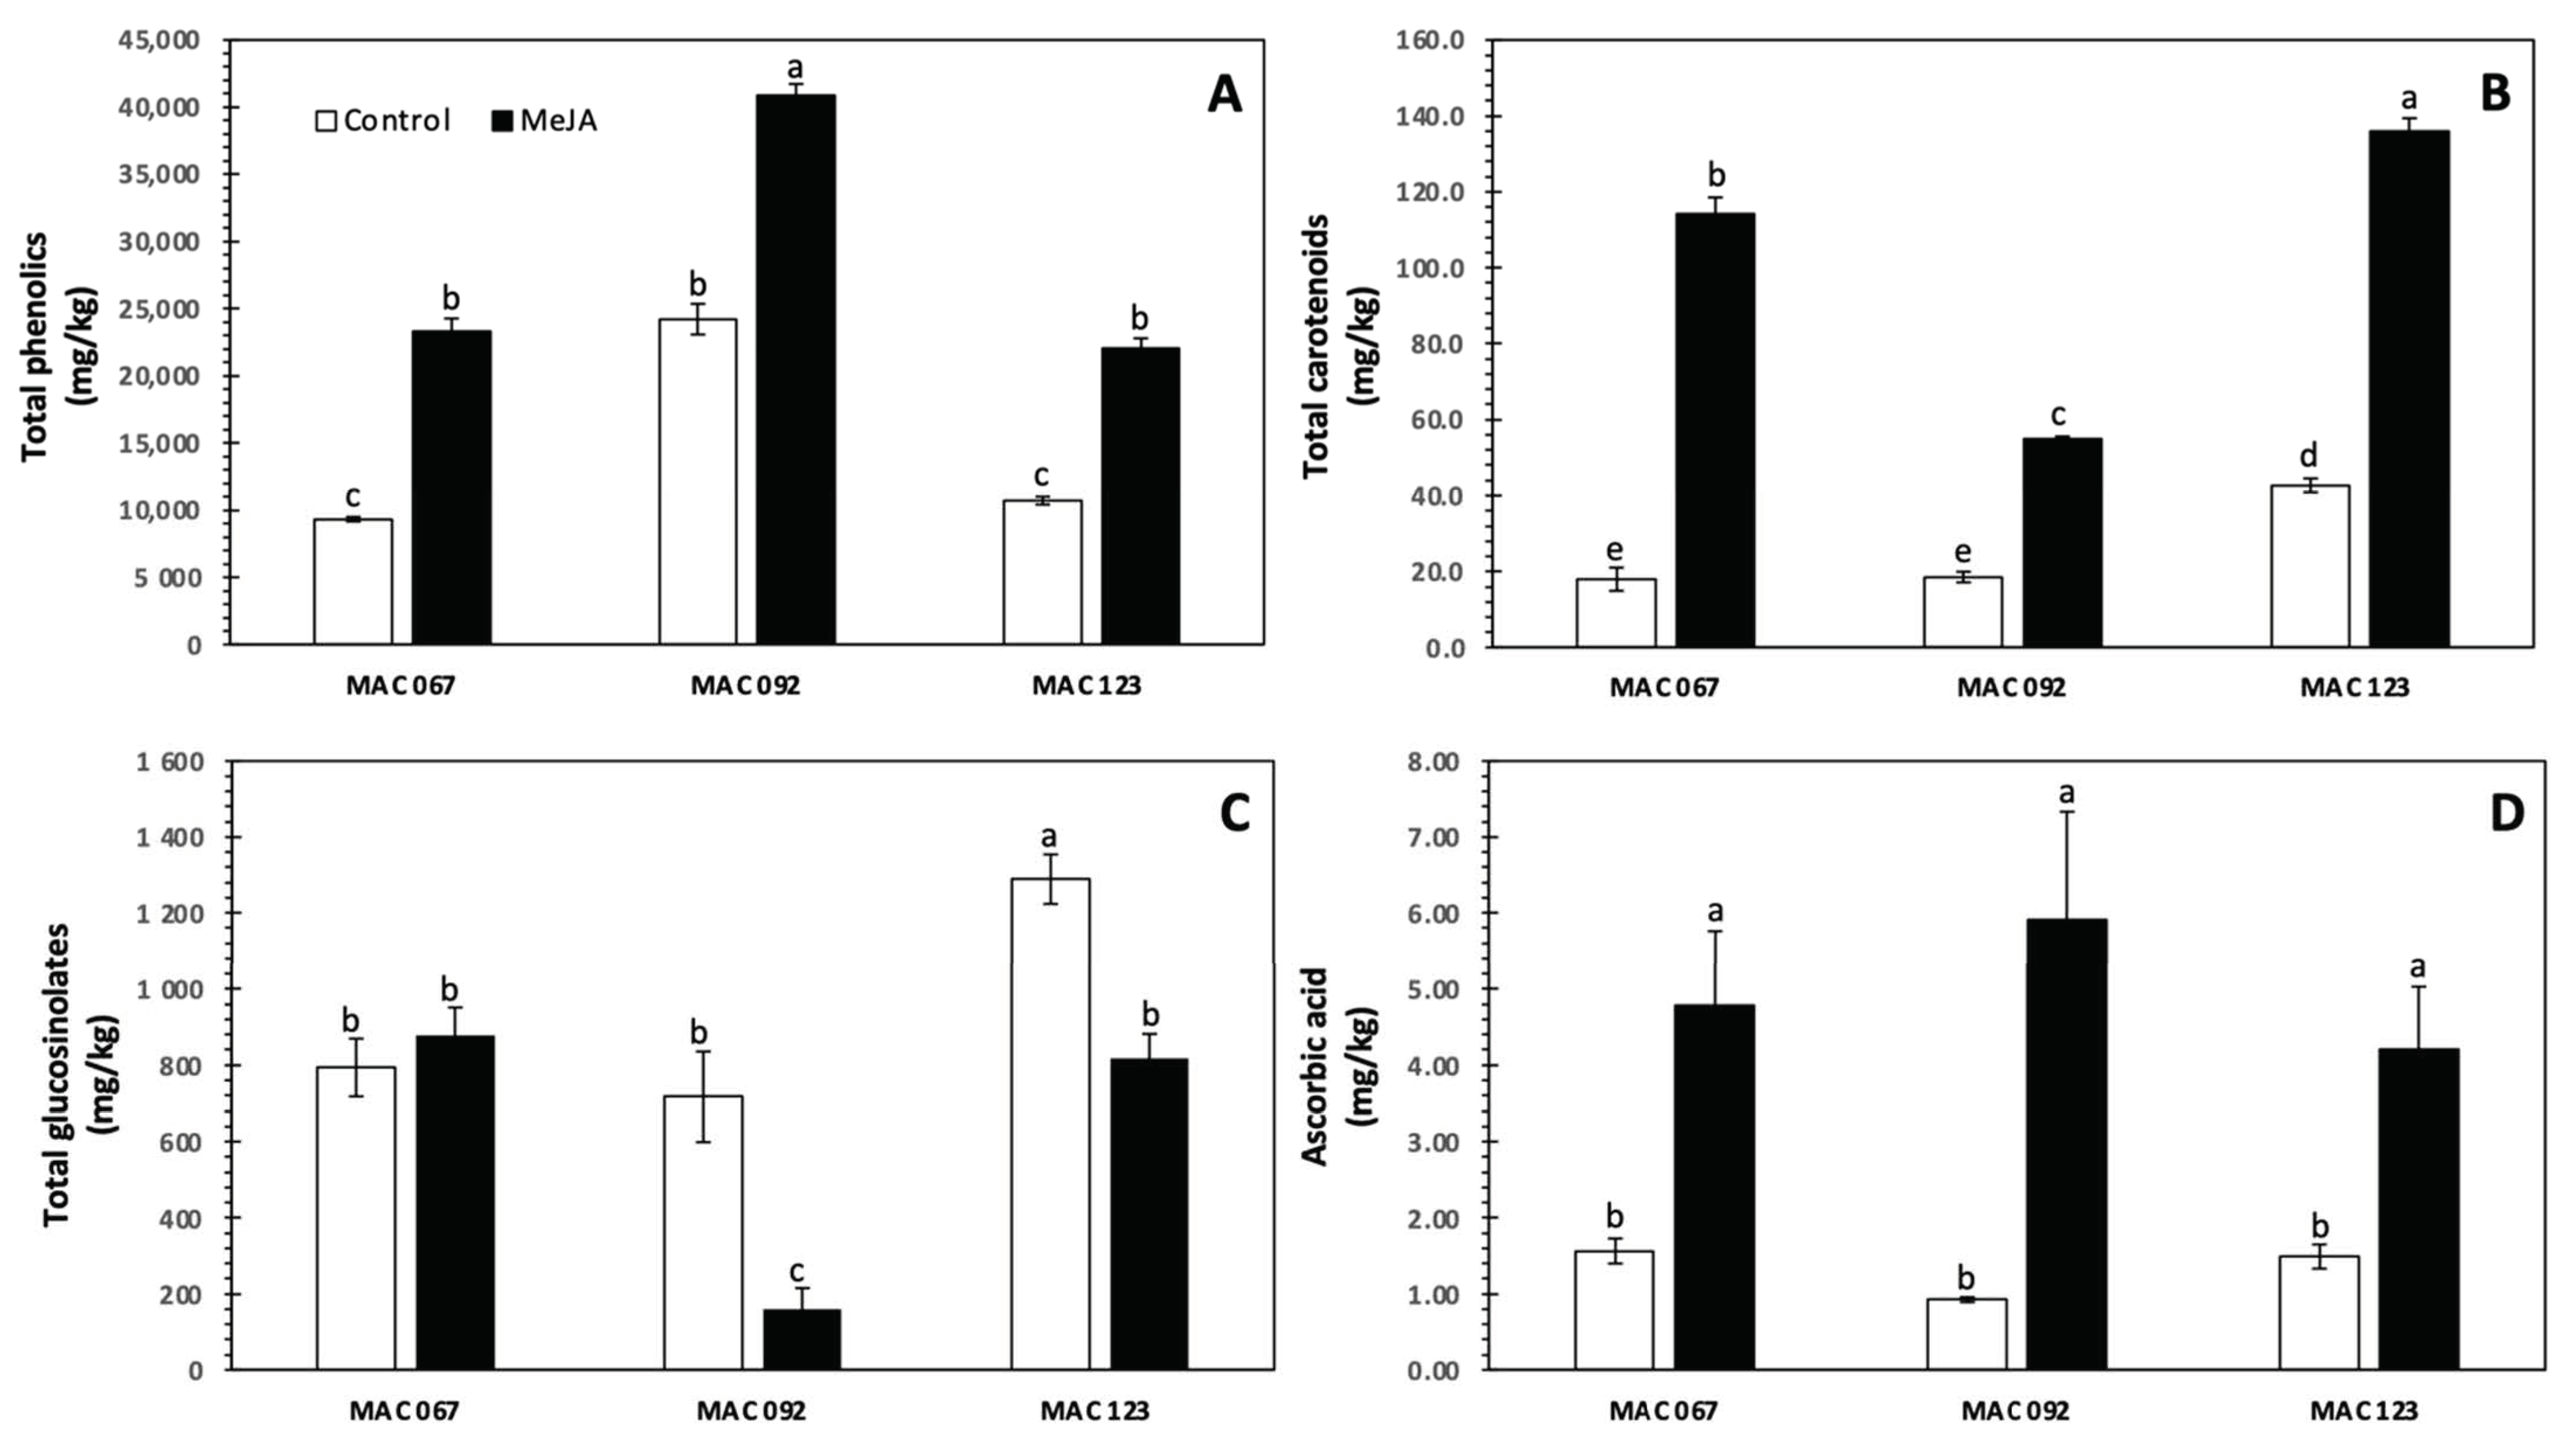
Three mashua morphotypes were selected to further evaluate the effect of MeJA on the accumulation of bioactive compounds (Figure 1). The morphotypes selected were those with the highest content of phenolics (MAC 092), glucosinolates (MAC 123), and with average levels of the bioactive compounds evaluated (MAC 067). For total phenolics, MeJA increased the total phenolics content by 150.1%, 68.7%, and 105.6% for MAC 067, MAC 092, and MAC 123 morphotypes, respectively. Indeed, the application of MeJA allowed MAC 067 and MAC 123 to reach the phenolic content of MAC 092, which was the morphotype identified with the highest concentration of phenolics (Figure 1A). These results agree with previous reports, where MeJA increased the content of phenolics in Brassica species such as Brassica rapa, kale leaves, broccoli florets, and broccoli sprouts [11,24,27,28,29], as well as in carrots [10].
Figure 1.
Effect of postharvest methyl jasmonate application on the accumulation of total phenolics (A); total carotenoids (B); total glucosinolates (C); and ascorbic acid (D) of Peruvian mashua accessions. Values represent the means of 3 replicates ± standard error. Different letters among bars indicate a statistical difference between the treatments using the LSD test (p < 0.05).
Regarding total carotenoids, MeJA induced 535.0%, 195.7%, and 218.2% increases for MAC 067, MAC 092, and MAC 123 morphotypes, respectively, converting the tissue from a moderate to a good source of carotenoids (Figure 1B). The MeJA-induced biosynthesis of carotenoids has been previously reported for crops such as maize [30]. However, other reports in broccoli sprouts indicate that MeJA decreases carotenoids [24], indicating that MeJA response in horticultural crops is tissue dependent.
Regarding total glucosinolates, no significant difference in the concentration was detected for the MAC 067 morphotype, whereas for MAC 092 and MAC 123, the content decreased by −77.8% and −36.5%, respectively (Figure 1C). This could be attributed to the MeJA-induced activation of myrosinase, which converts glucosinolates to isothiocyanates, as previously reported for radish sprouts [31].
Ascorbic acid content was also increased by applying MeJA, obtaining 206.4%, 542.4%, and 182.5% higher levels for MAC 067, MAC 092, and MAC 123, respectively (Figure 1D). Interestingly, MeJA increased ascorbic acid content to similar levels in the three morphotypes evaluated. The MeJA-induced accumulation of ascorbic acid has been previously reported for crops such as Arabidopsis and tobacco Bright Yellow-2 (BY-2) suspension cells [32] and broccoli [33]. Although MeJA increased the ascorbic acid content in mashua, the levels reached are still moderate compared with the primary sources of vitamin C [24].
4. Conclusions
The results presented herein indicate that the different mashua morphotypes evaluated represent an excellent source of phenolics and glucosinolates, adequate levels of carotenoids, and low levels of vitamin C. Since phenolics and glucosinolates are highly antioxidants, mashua represents an unexploited plant food that could be highly useful to prevent chronic and degenerative diseases in the population. Further studies should detail the effect of methyl jasmonate on the phenolic and glucosinolate profile of mashua. Likewise, further investigations should determine the physiological and molecular basis, inducing the biosynthesis of secondary metabolites in mashua due to exogenous methyl jasmonate application. In addition, it would be interesting to characterize other bioactive compounds in mashua (i.e., dietary fiber, terpenoids, etc.) and to develop bioprocesses that could transform mashua into a food ingredient or processed foods highly accepted by consumers.
Author Contributions
Conceptualization, D.A.J.-V. and G.P.-R.; methodology, D.A.J.-V., G.P.-R., V.A.-A., L.E.P.-A., O.H.-C., A.M.T.-C.; formal analysis, D.A.J.-V., G.P.-R., L.E.P.-A. and A.M.T.-C.; investigation, D.A.J.-V., G.P.-R., V.A.-A., L.E.P.-A. and A.M.T.-C.; resources, D.A.J.-V. and G.P.-R.; data curation D.A.J.-V., G.P.-R., L.E.P.-A. and A.M.T.-C.; writing—original draft preparation, D.A.J.-V. and G.P.-R.; writing—review and editing, D.A.J.-V.; project administration, D.A.J.-V. and G.P.-R.; funding acquisition, D.A.J.-V. and G.P.-R. All authors have read and agreed to the published version of the manuscript.
Funding
This study was supported by funds from Tecnologico de Monterrey (Bioprocess Research Group), and by the Ministry of Education (MINEDU) and the National Council of Science, Technology and Technological Innovation from Perú (CONCYTEC), through the Grant 199-2015-FONDECYT–UNSCH.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
The data presented in this study are available within the article.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Arbizu, C.; Tapia, M. Tubérculos andinos. In Cultivos Marginados: Otra Perspectiva de 1492; Hernández Bermajo, J.E., León, S., Eds.; Food and Agriculture Organization of the United Nations: Rome, Italy, 1992; pp. 147–161. [Google Scholar]
- Chirinos, R.; Campos, D.; Costa, N.; Arbizu, C.; Pedreschi, R.; Larondelle, Y. Phenolic profiles of andean mashua (Tropaeolum tuberosum Ruíz & Pavón) tubers: Identification by HPLC-DAD and evaluation of their antioxidant activity. Food Chem. 2008, 106, 1285–1298. [Google Scholar] [CrossRef] [Scilit]
- Inostroza, L.A.; Castro, A.J.; Hernández, E.M.; Carhuapoma, M.; Yuli, R.A.; Collado, A.; Córdova, J.S. Actividad antioxidante de Tropaeolum tuberosum Ruiz & Pavón (mashua) y su aplicación como colorante para yogur. Cienc. E Investig. 2015, 18, 83–89. [Google Scholar] [CrossRef] [Scilit]
- Quispe, C.; Mansilla, R.; Chacón, A.; Blas, R. Análisis de la variabilidad morfológica del “Añu” Tropaeolum tuberosum Ruiz & Pavón procedente de nueve distritos de la región Cusco. Ecol. Appl. 2015, 14, 211–222. [Google Scholar]
- Pissard, A.; Arbizu, C.; Ghislain, M.; Bertin, R. Influence of geographical provenance on the genetic structure and diversity of the vegetatively propagated Andean tuber crop, mashua (Tropaeolum tuberosum), highlighted by intersimple sequence repeat markers and multivariate analysis methods. Int. J. Plant Sci. 2008, 169, 1248–1260. [Google Scholar] [CrossRef] [Scilit]
- Ortega, O.R.; Kliebenstein, D.J.; Arbizu, C.; Ortega, R.; Quiros, C.F. Glucosinolate survey of cultivated and feral mashua (Tropaeolum tuberosum Ruiz & Pavón) in the Cuzco region of Peru. Econ. Bot. 2006, 60, 254–264. [Google Scholar] [CrossRef] [Scilit]
- Ticona, L.N.A.; Pérez, V.T.; Benito, P.B. Local/traditional uses, secondary metabolites and biological activities of Mashua (Tropaeolum tuberosum Ruíz & Pavón). J. Ethnopharmacol. 2020, 247, 112152. [Google Scholar] [CrossRef] [Scilit]
- Cisneros-Zevallos, L.; Jacobo-Velázquez, D.A. Controlled abiotic stresses revisited: From homeostasis through hormesis to extreme stresses and the impact on nutraceuticals and quality during pre- and postharvest applications in horticultural crops. J. Agric. Food Chem. 2020, 68, 11877–11879. [Google Scholar] [CrossRef] [Scilit]
- Jacobo-Velázquez, D.A. Definition of biofortification revisited. ACS Food Sci. Technol. 2022, 2, 782–783. [Google Scholar] [CrossRef] [Scilit]
- Heredia, J.B.; Cisneros-Zevallos, L. The effect of exogenous ethylene and methyl jasmonate on pal activity, phenolic profiles and antioxidant capacity of carrots (Daucus carota) under different wounding intensities. Postharvest Biol. Technol. 2009, 51, 242–249. [Google Scholar] [CrossRef] [Scilit]
- Villarreal-García, D.; Nair, V.; Cisneros-Zevallos, L.; Jacobo-Velázquez, D.A. Plants as biofactories: Postharvest stress-induced accumulation of phenolic compounds and glucosinolates in broccoli subjected to wounding stress and exogenous phytohormones. Front. Plant Sci. 2016, 7, 45. [Google Scholar] [CrossRef] [Scilit]
- Swain, T.; Hillis, W.E. The phenolics constituents of Prunus domestica. I. The quantitative analysis of phenolics constituents. J. Sci. Food Agric. 1959, 10, 63–68. [Google Scholar] [CrossRef] [Scilit]
- Sánchez-Rangel, J.C.; Benavides, J.; Heredia, J.B.; Cisneros-Zevallos, L.; Jacobo-Velázquez, D.A. The Folin–Ciocalteu assay revisited: Improvement of its specificity for total phenolic content determination. Anal. Methods 2013, 5, 5990–5999. [Google Scholar] [CrossRef] [Scilit]
- Cuéllar-Villarreal, M.R.; Ortega-Hernández, E.; Becerra-Moreno, A.; Welti-Chanes, J.; Cisneros-Zevallos, L.; Jacobo-Velázquez, D.A. Effects of ultrasound treatment and storage time on the extractability and biosynthesis of nutraceuticals in carrot (Daucus carota). Postharvest Biol. Technol. 2016, 119, 18–26. [Google Scholar] [CrossRef] [Scilit]
- Gross, J. Pigments in Vegetables: Chlorophylls and Carotenoids; Springer: New York, NY, USA, 1991. [Google Scholar]
- Gillespie, K.M.; Ainsworth, E.A. Measurement of reduced, oxidized and total ascorbate content in plants. Nat. Protoc. 2007, 2, 871–874. [Google Scholar] [CrossRef] [Scilit]
- Jacobo-Velázquez, D.A.; Cisneros-Zevallos, L. Correlations of antioxidant activity against phenolic content revisited: A new approach in data analysis for food and medicinal plants. J. Food Sci. 2009, 74, R107–R113. [Google Scholar] [CrossRef] [Scilit]
- Chirinos, R.; Campos, D.; Betalleluz, I.; Giusti, M.M.; Schwartz, J.; Tian, Q.; Pedreschi, R.; Larondelle, Y. High-performance liquid chromatography with photodiode array detection (HPLC−DAD)/HPLC−mass spectrometry (MS) profiling of anthocyanins from Andean mashua tubers (Tropaeolum tuberosum Ruíz and Pavón) and their contribution to the overall antioxidant activity. J. Agric. Food Chem. 2006, 54, 7089–7097. [Google Scholar] [CrossRef] [Scilit]
- Velioglu, Y.S.; Gao, M.L.; Oomah, B.D. Antioxidant activity and total phenolics in selected fruits, vegetables, and grain products. J. Agric. Food Chem. 1998, 46, 4113–4117. [Google Scholar] [CrossRef] [Scilit]
- Chun, O.K.; Kim, D.-O. Consideration on equivalent chemicals in total phenolic assay of chlorogenic acid-rich plums. Food Res. Int. 2004, 37, 337–342. [Google Scholar] [CrossRef] [Scilit]
- Edge, R.; Truscott, T.G. Singlet oxygen and free radical reactions of retinoids and carotenoids—A review. Antioxidants 2018, 7, 5. [Google Scholar] [CrossRef] [Scilit]
- Fahey, J.W.; Zalcmann, A.T.; Talalay, P. The chemical diversity and distribution of glucosinolates and isothiocyanates among plants. Phytochemistry 2001, 56, 5–51. [Google Scholar] [CrossRef] [Scilit]
- Halkier, B.A.; Gershenzon, J. Biology and biochemistry of glucosinolates. Annu. Rev. Plant Biol. 2006, 57, 303–333. [Google Scholar] [CrossRef] [Scilit]
- Moreira-Rodríguez, M.; Nair, V.; Benavides, J.; Cisneros-Zevallos, L.; Jacobo-Velázquez, D.A. UVA, UVB light, and methyl jasmonate, alone or combined, redirect the biosynthesis of glucosinolates, phenolics, carotenoids, and chlorophylls in broccoli sprouts. Int. J. Mol. Sci. 2017, 18, 2330. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fenech, M.; Amaya, I.; Valpuesta, V.; Botella, M.A. Vitamin C content in fruits: Biosynthesis and regulation. Front. Plant Sci. 2019, 9, 2006. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Park, W.T.; Kim, Y.B.; Seo, J.M.; Kim, S.J.; Chung, E.; Lee, J.H.; Park, S.U. Accumulation of anthocyanin and associated gene expression in radish sprouts exposed to light and methyl jasmonate. J. Agric. Food Chem. 2013, 61, 4127–4132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pérez-Balibrea, S.; Moreno, D.A.; García-Viguera, C. Improving the phytochemical composition of broccoli sprouts by elicitation. Food Chem. 2011, 129, 35–44. [Google Scholar] [CrossRef] [Scilit]
- Ku, K.M.; Juvik, J.A. Environmental stress and methyl jasmonate-mediated changes in flavonoid concentrations and antioxidant activity in broccoli florets and kale leaf tissues. HortScience 2013, 48, 996–1002. [Google Scholar] [CrossRef] [Scilit]
- Ku, K.M.; Jeffery, E.H.; Juvik, J.A. Influence of seasonal variation and methyl jasmonate mediated induction of glucosinolate biosynthesis on quinone reductase activity in broccoli florets. J. Agric. Food Chem. 2013, 61, 9623–9631. [Google Scholar] [CrossRef] [Scilit]
- Lou, H.; He, W.; Li, D.; Bao, Y.; Riaz, A.; Xiao, Y.; Song, J.; Liu, C. Effect of methyl jasmonate on carotenoids biosynthesis in germinated maize kernels. Food Chem. 2020, 307, 125525. [Google Scholar] [CrossRef] [Scilit]
- Kim, H.-J.; Chen, F.; Wang, X.; Choi, J.-H. Effect of methyl jasmonate on phenolics, isothiocyanate, and metabolic enzymes in radish sprout (Raphanus sativus L.). J. Agric. Food Chem. 2006, 54, 7263–7269. [Google Scholar] [CrossRef] [Scilit]
- Wolucka, B.A.; Goossens, A.; Inzé, D. Methyl jasmonate stimulates the de novo biosynthesis of vitamin C in plant cell suspensions. J. Exp. Bot. 2005, 56, 2527–2538. [Google Scholar] [CrossRef] [Scilit]
- Aguilar-Camacho, M.; Welti-Chanes, J.; Jacobo-Velázquez, D.A. Combined effect of ultrasound treatment and exogenous phytohormones on the accumulation of bioactive compounds in broccoli florets. Ultrason. Sonochem. 2019, 50, 289–301. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).