Article

Phylogeographic Insights into Aedes albopictus in Korea: Integrating COX1, ND5, and CYTB Analyses
1
Department of Biomedical Laboratory Science, College of Software and Digital Healthcare Convergence, Yonsei University, Wonju 26493, Republic of Korea
2
One Health Frontiers, Co., Ltd., Wonju 26493, Republic of Korea
3
Department of Medical Environmental Biology and Tropical Medicine, School of Medicine, Kangwon National University, Chuncheon 24341, Republic of Korea
4
Department of Epidemiology and Tropical Diseases, Faculty of Public Health, Universitas Diponegoro, Semarang 50275, Indonesia
5
Division of Zoonotic and Vector Borne Disease Research, Center for Infectious Diseases Research, Korea National Institute of Health, Cheongju 28159, Republic of Korea
*
Authors to whom correspondence should be addressed.
These authors contributed equally to this work.
Insects 2026, 17(1), 82; https://doi.org/10.3390/insects17010082
Submission received: 13 October 2025 / Revised: 30 December 2025 / Accepted: 7 January 2026 / Published: 10 January 2026
(This article belongs to the Special Issue Challenges in Mosquito Surveillance and Control)

Simple Summary

The Asian tiger mosquito (Aedes albopictus) is an invasive species that can spread medically important arboviruses such as dengue, chikungunya, and Zika. Its ability to expand worldwide is strongly influenced by climate change and human travel. In South Korea, this mosquito is widely distributed, but few studies have integrated multiple mitochondrial markers. In this study, we collected mosquitoes from 13 locations in seven provinces and analyzed their genetic material using three markers: COX1, ND5, and CYTB, which are useful for tracing the relationship among mosquito populations and understanding how they may spread between regions. Our results showed high genetic diversity in southern coastal areas such as Busan and Suncheon, suggesting these regions may serve as entry points for new introductions. The findings also revealed distinct groups in mainland Korea and Jeju Island. Using multiple genetic markers provided an understanding of mosquito diversity and their links to international populations, supporting mosquito surveillance and effective control strategies for Ae. albopictus in Korea and beyond.

Abstract

The Asian tiger mosquito (Aedes albopictus) is an important vector of arboviruses, including dengue, chikungunya, and Zika. Its rapid global expansion has been facilitated by climate change and human activities. Phylogenetic studies of Ae. albopictus have largely relied on mitochondrial cytochrome c oxidase subunit 1 (COX1) and NADH dehydrogenase subunit 5 (ND5) markers, while the utility of cytochrome b (CYTB) remains underexplored. We collected Ae. albopictus from 13 sites in seven provinces of South Korea and analyzed COX1, ND5, and CYTB sequences. Genetic diversity indices were calculated, and phylogenetic relationships were reconstructed using maximum-likelihood trees and haplotype networks with a dataset obtained from GenBank. COX1 revealed 46 haplotypes, including six novel variants, with the highest diversity in southern coastal regions such as Busan and Suncheon. ND5 showed limited variation, with only two haplotypes. CYTB revealed three haplotypes, including region-specific variants in Busan and Wonju, supporting its role as a complementary marker. The Busan haplotype H41 bridged domestic and international lineages, suggesting Busan as a likely entry point. This study demonstrates that integrating COX1, ND5, and CYTB improves the resolution of Ae. albopictus phylogeography in Korea and highlights the need for continued molecular surveillance to guide vector control strategies.

1. Introduction

Vector-borne diseases transmitted by arthropods such as mosquitoes, ticks, and sandflies remain a major public health concern. Climate change—particularly increases in global temperatures, altered rainfall patterns, and rising humidity—affects their transmission by enhancing the survival, reproduction, and geographic expansion of vectors [1,2]. Dengue fever is endemic in tropical and subtropical regions, and its spread is driven by climate change, rapid urbanization, and increasing population density [3]. A notable dengue outbreak in Japan in 2014, despite having no prior history of dengue outbreaks [4]. Chikungunya, originally endemic to Africa, was first reported outside the continent during an outbreak in Italy in 2007 [5], and has since spread across tropical and subtropical regions in Europe, Asia, and South America, causing multiple epidemics with increasing frequency [6]. In Korea, malaria and Japanese encephalitis remain the primary mosquito-borne diseases of concern [7]. Imported cases of dengue, chikungunya, and Zika virus infections continue to be reported [8], raising concern about the potential introduction and establishment of these diseases [9].
Major vectors capable of transmitting arboviruses such as dengue, Zika, and chikungunya include Yellow fever mosquito (Aedes aegypti, Ae. aegypti) and the Asian tiger mosquito (Ae. albopictus). The Ae. aegypti mosquito is highly anthropophilic, breeding primarily in artificial containers around human dwellings, and is a major vector of dengue fever, Zika virus, chikungunya virus, and yellow fever [8]. Ae. aegypti is widely distributed across tropical and subtropical regions, including Africa, the Americas, South and Southeast Asia, and the Pacific islands. However, its distribution is significantly constrained by temperature and humidity because it relies heavily on human habitats and relatively warm environments [10].
By contrast, the Asian tiger mosquito (Ae. albopictus), native to Asian forests, is more ecologically versatile [11]. It can utilize both natural and artificial containers, tolerate a broader range of climates, and establish itself in peri-urban and rural environments. Like Ae. aegypti, it is a competent vector of multiple arboviruses, but it is considered far more invasive [12]. Since the 1980s, Ae. albopictus has expanded rapidly into the Americas, Europe, and many Pacific islands. The ability of temperate Ae. albopictus strains to survive freezing temperatures and overwinter as diapausing eggs has facilitated its establishment in cooler temperate regions where Ae. aegypti cannot persist [13]. The continued global spread of Ae. albopictus underscores the growing potential for arboviral transmission at higher latitudes [2,14].
Determining the routes of mosquito introduction is critical for understanding the global spread of invasive vector species. Phylogenetic analysis has been employed to investigate the population structure of mosquitoes, identify distinct haplotypes, and elucidate both regional differentiation and international genetic relationships. For this purpose, mitochondrial DNA has been widely employed in phylogenetic studies owing to its maternal inheritance and relatively rapid mutation rate [15]. The mitochondrial genome of Ae. albopictus is 16,665 bp in length, and the COX1 (cytochrome c oxidase subunit 1) gene is among the most frequently used markers for phylogenetic analyses, owing to its standard barcode region, high mitochondrial mutation rate, and strong discriminatory power [16]. Phylogenetic analyses using the COX1 gene have provided evidence for the species’ recent global expansion [17]. NADH dehydrogenase subunit 5 (ND5) has been reported as a useful marker for population and geographical phylogenetic analyses of Ae. albopictus in Malaysia [18] as well as in Cameroon, Hawaii, Brazil, and the United States [19]. However, a study by Palacio-Cortés in Brazil reported a relatively low ND5 genetic diversity [20]. Cytochrome b (CYTB) is a useful phylogenetic marker across insects, including mosquitoes [21], and has been used to analyze population structure and patterns in other mosquito genera, including Anopheles and Culex [22]. In Ae. albopictus, a phylogenetic study of Mexican populations using CYTB revealed substantial genetic variation and provided insights into invasion pathways [23], whereas other studies have reported relatively low CYTB diversity in this species [18].
In Korea, phylogeographic analyses of Ae. albopictus have primarily relied on COX1 sequences [24,25]. Although recent studies have incorporated both COX1 and ND5, the phylogenetic resolution of ND5 remains unclear [25], and no studies have evaluated CYTB in Korean Ae. albopictus populations. Phylogenetic investigations of the introduction routes of Ae. albopictus population in Korea are still limited.
Therefore, in this study, we assessed the phylogeographic utility of CYTB—together with ND5 and COX1—for Ae. albopictus populations in Korea and used these markers to investigate the geographic invasion into Korea.

2. Materials and Methods

2.1. Mosquito Collection and Identification

To investigate the genetic diversity of Asian tiger mosquitoes (Ae. albopictus) in the Republic of Korea, adult mosquitoes were collected from 13 sites across seven provinces. A portion of the specimens was obtained through the mosquito-borne disease surveillance program conducted by the Korea Centers for Disease Control and Prevention (KDCA). Mosquitoes were collected from 15:00 to 10:00 (overnight) using BG-Sentinel™ traps (Biogents AG, Regensburg, Germany) baited with BG-Lure® and carbon dioxide supplied via dry ice.
The collection sites were as follows: Chuncheon, Donghae, Gangneung, Samcheok, Sokcho, and Wonju in Gangwon Province; Dangjin, and Geumsan in Chungnam Province; Chungju in Chungbuk Province; Suncheon in Jeonnam Province; Jinju in Gyeongnam Province; and Goryeong in Gyeongbuk Province, and Busan Metropolitan City (Table S1).
A total of 4658 adult mosquitoes were collected and morphologically identified to species level by light microscopy using the taxonomic key described by Ree [26] (Table S1). Of the 542 Ae. albopictus collected, 54 individuals were selected for genetic analyses to ensure high-quality DNA and balanced regional representation.

2.2. Ethical Approval

All procedures involving the collection and handling of mosquitoes were reviewed and approved by the Institutional Animal Care and Use Committee (IACUC) of Yonsei University Mirae Campus (Approval No. YWCI-202005-007-02). All experiments were conducted in accordance with the IACUC guidelines.

2.3. DNA Extraction, PCR Amplification, and Sequencing

Mosquitoes morphologically identified as Ae. albopictus were washed twice in 70% ethanol and placed into reinforced homogenizing tubes (Bertin, Montigny-le-Bretonneux, France) containing 2.8 mm zirconium oxide beads (Bertin) and 200 μL of TRIzol reagent (Invitrogen, Waltham, MA, USA). Mosquitoes were chilled at 4 °C for 30 min prior to homogenization, and homogenized twice at 5000 rpm for 20 s using a mechanical homogenizer (Precellys Evolution Touch Homogenizerl, Bertin Technologies, Montigny-le-Bretonneux, France). Genomic DNA was extracted using the G-spin™ Total DNA Extraction Mini Kit (Intron Biotechnology Inc., Seongnam, Republic of Korea) according to the manufacturer’s instructions and stored at −80 °C until further use.
To analyze the genetic diversity of Ae. albopictus, variable regions of three mitochondrial genes—COX1, ND5, and CYTB—were targeted [27,28]. Primers newly designed using Primer3 software (https://bioinfo.ut.ee/primer3-0.4.0 (accessed on 5 May 2020)) were used to amplify COX1 (nucleotide positions 2219–2966) and the CYTB (10,426–10,963) of the GenBank mitochondrial genome of Ae. albopictus (GenBank accession no. NC_006817) (Table S1).
PCR amplification was performed in a total volume of 20 μL using the AccuPower® PCR PreMix kit (Bioneer Co., Daejeon, Republic of Korea), which contains Taq DNA polymerase and dNTPs, with 2 μL of each primer (10 pmol/μL), 2 μL of template DNA, and 14 μL of distilled water. PCR amplification conditions for COX1 and ND5 consisted of an initial denaturation at 95°C for 5 min, followed by 35 cycles of 94 °C for 30 s, 55 °C for 60 s, and 72 °C for 60 s, with a final extension at 72 °C for 7 min. For CYTB, amplification was performed with an initial denaturation at 95 °C for 10 min, followed by 35 cycles of 95 °C for 30 s, 60 °C for 60 s, and 72 °C for 30 s, and a final extension at 72°C for 7 min. PCR products were separated on a 1.5% agarose gel by electrophoresis at 180 V for 30 min. The amplified fragments were purified using the LaboPass™ Gel and PCR Clean-up Kit (Cosmo Genetech Co., Seoul, Republic of Korea) and sequenced with the ABI Prism BigDye (ThermoFisher Scientific Inc., Waltham, MA, USA) by Macrogen (Macrogen Inc., Seoul, Republic of Korea).

2.4. Sequence Editing and Alignment

The amplified sequences of the mitochondrial genes COX1, ND5, and CYTB were inspected using ChromasPro (version 2.1.9, Technelysium Pty Ltd., South Brisbane, Australia), and low-quality base calls at the 5′ and 3′ ends were trimmed using BioEdit (version 7.2, Ibis Biosciences Co., Carlsbad, CA, USA). Forward and reverse reads were assembled into consensus sequences. Consensus sequences were aligned using MEGA X (version 10.2.6, megasoftware.net) with the MUSCLE algorithm [29], applying default gap-opening and gap-extension penalties. After alignment, all sequence fragments were trimmed to equal lengths for phylogenetic and haplotype network analyses.

2.5. Phylogenetic Analysis

Phylogenetic trees based on the aligned sequences retrieved from GenBank and those generated in this study were constructed using the maximum likelihood method under the Tamura–Nei model with 1,000 bootstrap replicates implemented in MEGA X [30].

2.6. Genetic Variation and Haplotype Network Analysis

Sequence comparison was conducted using the Needleman–Wunsch algorithm and the Smith–Waterman algorithm [31,32]. Population nucleotide diversity indices such as number of haplotypes, haplotype diversity (Hd), nucleotide diversity per site (π), average number of nucleotide differences (k), and number of polymorphic sites (S) were calculated using DnaSP (ver. 6.12.03, University of Barcelona, Spain) [33]. The haplotypes of the COX1 gene of Ae. albopictus were classified based on the KDCA study as a reference [26]. The pairwise distance of the haplotypes of Ae. albopictus was calculated using the MEGA X program.
The PopArt 1.7 (ver. 1.7, University of Otago, New Zealand) was used to construct a median-joining haplotype network analysis based on the region or country of source of Ae. albopictus to estimate the relationship between haplotypes using nexus input files produced by DnaSP version 6.12.03 [34].

3. Results

3.1. Genetic Differentiation and Diversity

To investigate the genetic diversity of Ae. albopictus populations, sequences of three mitochondrial genes (COX1, ND5, and CYTB) were aligned with datasets retrieved from GenBank. Two COX1 sequences (694 bp and 653 bp) were obtained from Korean Ae. albopictus were trimmed and aligned, and combined produce 48 sequence fragments with a total length of 1,347 bp. Additionally, 46 ND5 trimmed sequences (406 bp) and 47 CYTB trimmed sequences (472 bp) were aligned with corresponding GenBank data.

3.1.1. Genetic Diversity of Ae. albopictus Based on COX1

Forty-eight COX1 sequences (1347 bp) of Korean Ae. albopictus were aligned, and haplotypes and genetic variation indices were analyzed, including COX1 sequences previously reported in Korea (Table 1). Analysis of the Korean COX1 sequences revealed nine haplotypes, six of which (H39–H44) were newly identified in this study. The H1 haplotype was predominant, occurring in 38 of the 48 sequences (79.2%).
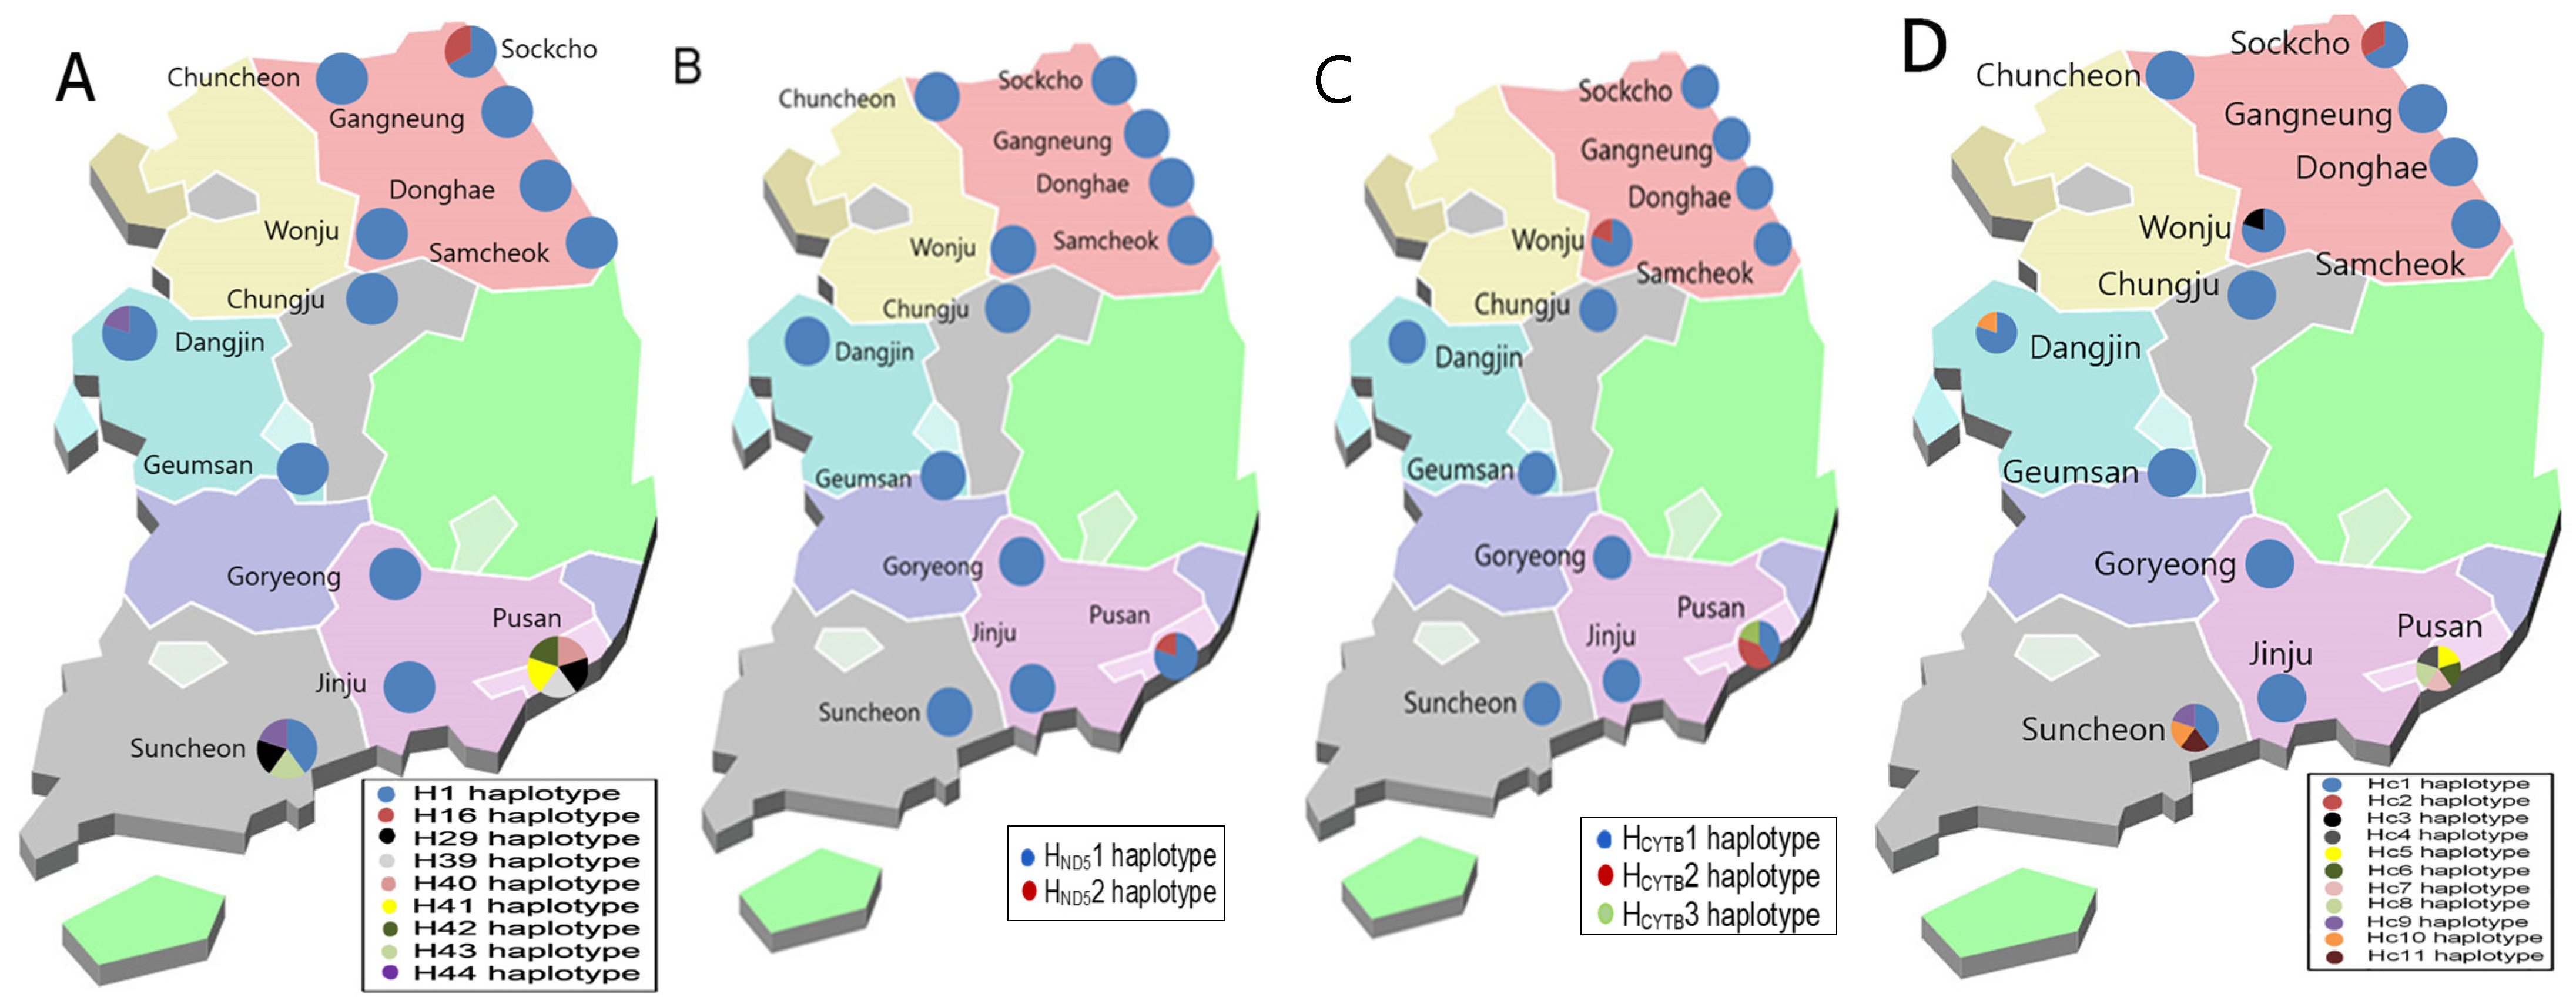
Regional haplotype distribution showed that most regions harbored a single dominant haplotype (H1) (Figure 1A). Notably, Busan exhibited the highest haplotype diversity, with five distinct haplotypes (Hd = 1.000), followed by Suncheon with four haplotypes (Hd = 0.900), and Sokcho with two (Hd = 0.667). Genetic diversity was detected nationwide, with particularly high variation observed in the southern coastal region, including Busan and Suncheon.

3.1.2. Genetic Diversity of Ae. albopictus Based on ND5 and CYTB

Analysis of mitochondrial ND5 and CYTB sequences revealed low overall genetic diversity in Korean Ae. albopictus, with most variation concentrated in Busan and, to a lesser extent, Wonju (Table 2 and Table 3).
Across 46 ND5 sequences, only two haplotypes were identified, with HND51 overwhelmingly dominant (97.8%) and HND52 detected only in Busan. This indicates that ND5 variation is extremely limited and confined to specific regions. This contrasts with COX1, which showed broader variability across regions.
Similarly, CYTB analysis of 47 sequences revealed only 3 haplotypes, with HCYTB1 accounting for 93.6% of all samples. Additional haplotypes were observed only in Busan and Wonju, particularly Wonju, where COX1 showed no variation, but CYTB revealed distinct diversity. Although ND5 did not provide additional genetic diversity beyond that detected by COX1, CYTB exhibited higher diversity than COX1 in a certain region, suggesting that a multi-locus approach incorporating COX1 may be advantageous for assessing genetic diversity.
Overall, the ND5 and CYTB analyses indicated that the Korean Ae. albopictus population showed limited nationwide diversity, with genetic variation exclusively restricted to a specific region—especially Busan.

3.1.3. Genetic Diversity of Ae. albopictus Based on Concatenated Sequences of COX1, ND5, and CYTB

To access the genetic diversity of the Korean Ae. albopictus, mitochondrial sequences of COX1, ND5, and CYTB were concatenated and analyzed. A total of 46 concatenated sequences were obtained, and 11 haplotypes (Hc1—Hc11) were identified (Table 4). The Hc1 haplotype was predominant and widely distributed nationwide. Moderate genetic diversity was observed in some regions, such as Sokcho and Wonju, where two haplotypes were detected. The highest diversity (Hd = 0.571) was observed in the southern coastal region. Busan exhibited the greatest haplotype richness, with five distinct haplotypes (Hc4—Hc8), all of which were unique to this region. Similarly, Suncheon showed relatively high genetic diversity, harboring four haplotypes (Hc1, Hc9, Hc10, and Hc11).
Overall, the concatenated mitochondrial datasets represent a key methodological advancement, providing greater discriminatory power than COX1-only analyses and enabling improved resolution of regional genetic variation and rare haplotypes.

3.2. Pairwise Genetic Distance of Ae. albopictus

3.2.1. Pairwise Genetic Distance of Ae. albopictus Based on the COX1 Gene

Pairwise genetic distances between Korean Ae. albopictus COX1 haplotypes and a foreign haplotype from a dataset containing 28 sequences were analyzed (Table S3). Several Italian haplotypes were identical to the Korean H41 haplotype and were grouped accordingly. Within Korea, COX1 genetic distances were low (0.0000–0.0037), with the greatest divergence occurring between H40 and H42–H44, and between H16 and H40—both H40 and H42 being detected in Busan. The dominant haplotype H1 showed minimal divergence from most Korean haplotypes (0.0000–0.0022).
Between the regions, pairwise distances ranged from 0.0007 to 0.0098, with the highest values observed between Philippine haplotypes 1 and 4 and Taiwan. Relative to Korean haplotypes, H16, H42, and H43 showed the greatest divergence (0.0083) from Philippine haplotypes, followed by Taiwan (0.0060) and Thailand (0.0052). In contrast, genetic distances with neighboring populations from China (0.0007–0.0022) and Japan (0.0015–0.0037) were comparatively low.

3.2.2. Pairwise Genetic Distance of Ae. albopictus Based on the ND5 and CYTB Gene

Pairwise genetic distances were analyzed between Korean Ae. albopictus ND5 haplotypes and foreign haplotypes from a dataset containing 38 sequences obtained from global regions. All foreign sequences matched the predominant Korean haplotype HND51 (Table S4). ND5 genetic distances ranged from 0.0025 to 0.2018, with the highest divergence (0.2018) observed between Taiwan (NC006817.1) and both HND52 and the Brazilian haplotype, indicating a unique Taiwanese lineage. All other pairwise distances, including that between HND51 and HND52 (0.0025), were very low.
For CYTB, comparisons with foreign haplotypes containing 16 sequences from Asia, Europe, Africa, and the Americas showed that many international sequences were identical to the dominant Korean haplotype HCYTB1 (Table S5). CYTB genetic distances ranged from 0.0000 to 0.0275, with the highest values observed between the Philippine haplotype 4 and Hawaii (0.0275), and between Korean HCYTB3 and Cambodia (0.0255). Within Korea, CYTB distances were low (0.0002–0.0125), indicating limited intraspecific variation.

3.2.3. Pairwise Genetic Distance of Ae. albopictus Based on Concatenated Sequences of COX1, ND5, and CYTB

Pairwise genetic distances between haplotypes within Korean Ae. albopictus population, calculated by concatenating COX1, ND5, and CYTB sequences, were low, ranging from 0.0005 to 0.0032 (Table S6). The genetic distances between Korean haplotypes and those from other geographical regions were quite high. The highest genetic distance (0.0293–0.0312) was observed with the Taiwanese haplotype, while Southeast Asian populations, including the Philippines and Thailand, showed intermediate genetic distance.
Overall, pairwise distance analysis of concatenated mitochondrial sequence supports the usefulness of multi-locus mitochondrial data for resolving fine-scale phylogeographic relationships in the Asian tiger mosquito.

3.3. Haplotype Network Analysis

The haplotype network of Korean Ae. albopictus COX1, ND5, and CYTB sequences were analyzed using the TCS method, together with datasets obtained from GenBank. A total of 48 COX1, 46 ND5, and 47 CYTB sequences from Korean Ae. albopictus were included, along with 28, 39, and 16 foreign sequences for the respective genes.

3.3.1. Haplotype Network Analysis of Ae. albopictus Based on COX1

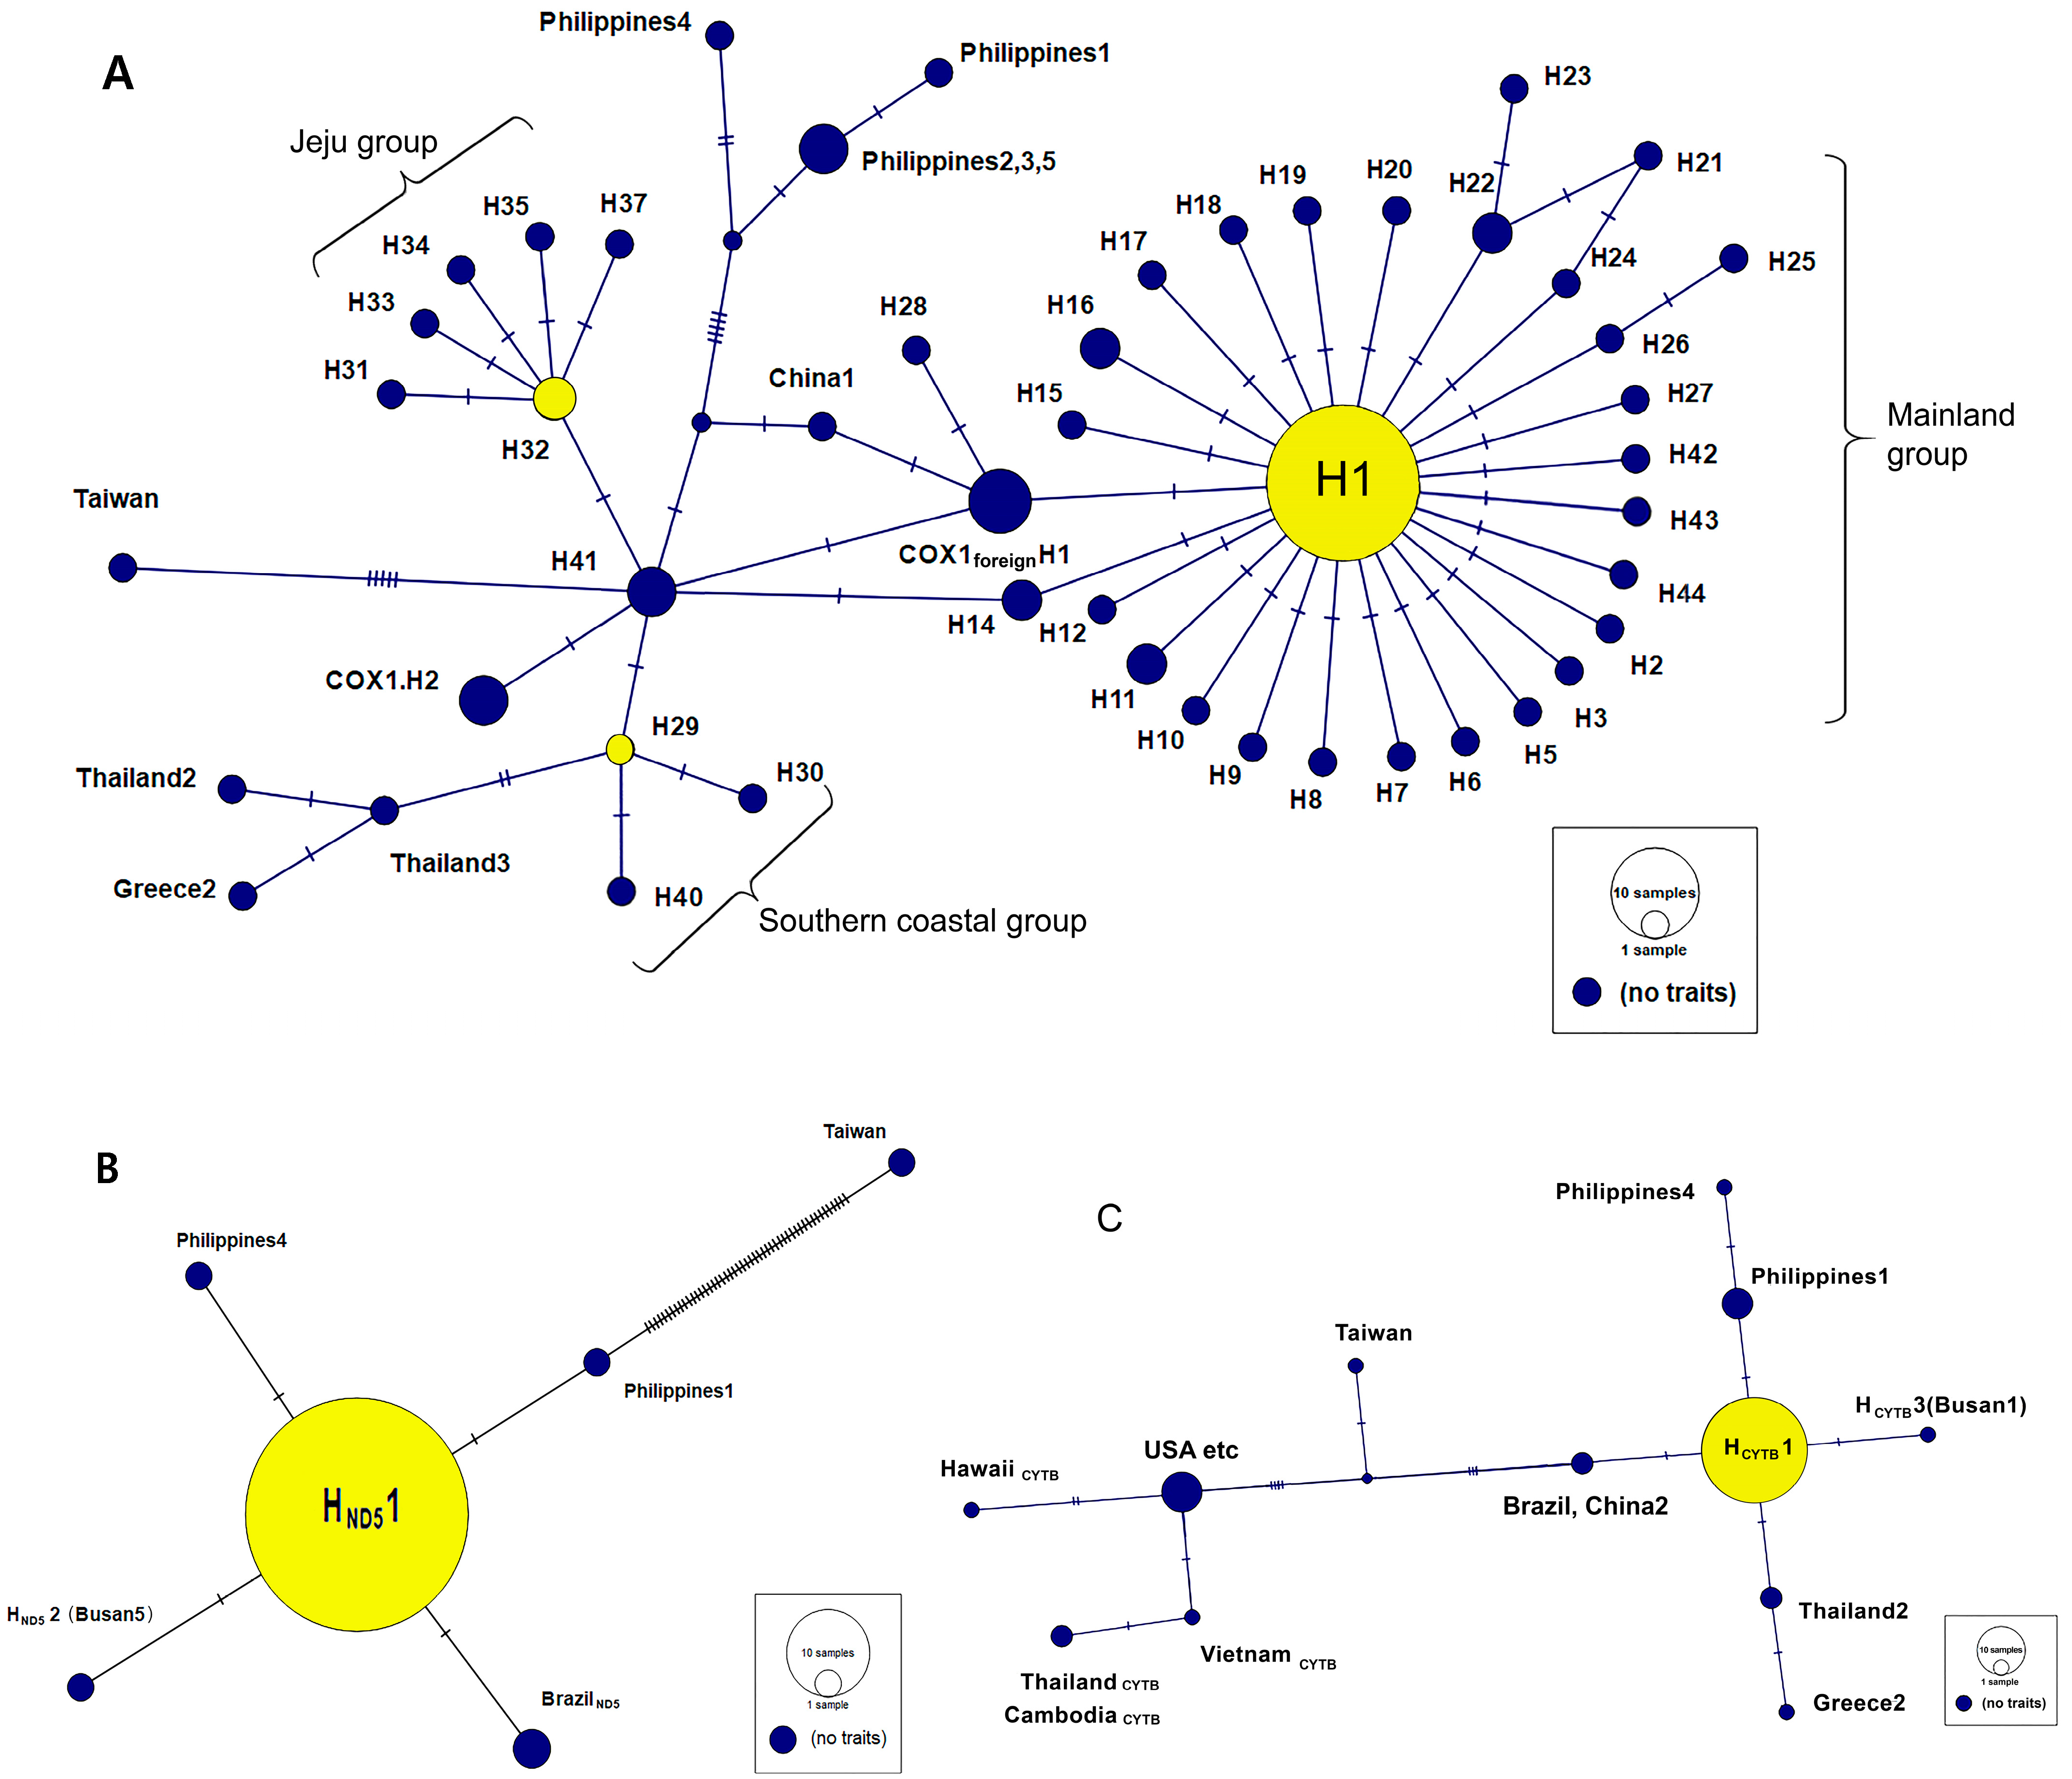
The haplotype network of Ae. albopictus was constructed using 1,347 bp COX1 sequences generated by trimming and merging two amplicons, together with previously reported domestic and international haplotypes, including those from Jeju Island (Figure 2A). The haplotype network revealed three distinct groups—mainland, southern coastal, and Jeju group. The mainland group was centered on the core H1 haplotype, surrounded by multiple satellite haplotypes (H2–H27, H39, and H42–H44), and was only one base pair from a foreign H1 haplotype containing sequences from Europe, China, and Brazil. The southern coastal group was organized around H29, with H30 and H40 branching from it, and connected by one base pair to a Thailand haplotype. The Jeju group formed an isolated cluster centered on H32 and H36. The H41 haplotype (Busan 4) served as a key connector, linking the southern coastal (H29), Jeju (H32, H36), and mainland (via H14) groups, and further connecting to haplotypes from China, Japan, the Philippines, Portugal, and Taiwan. The bridge haplotype H41, detected in Busan—a major international port—strongly supports a port-mediated introduction and dispersal hypothesis, indicating that marine trade and human-mediated transport have played a significant role in shaping the genetic structure of Ae. albopictus populations in Korea.

3.3.2. Haplotype Network Analysis of Ae. albopictus Based on ND5 and CYTB

A haplotype network of 87 ND5 sequences (397 bp) showed HND51 as the core haplotype, with the Korean HND52 and foreign haplotypes from the Philippines and Brazil differing by only one base pair. In contrast, the TaiwanND5 haplotype was highly divergent, separated from Philippine 1 by 48 base pairs (Figure 2B).
For CYTB, analysis of 47 Korean and 86 foreign sequences (Figure 2C) identified HCYTB1 as the central haplotype. HCYTB2 and HCYTB3 differed from HCYTB1 by one base pair, and HCYTB3 showed no direct connection to foreign haplotypes. HCYTB1 clustered with haplotypes from the Philippines, Thailand, and China, whereas Taiwan, Brazil, and the “USA–etc.” cluster (Brazil, France, Lebanon, USA) were positioned at much greater genetic distances. Southeast Asian haplotypes (Vietnam, Thailand, Cambodia) also grouped with this distant cluster, remaining well separated from Korean haplotypes.

3.3.3. Haplotype Network Analysis of Ae. albopictus Based on Concatenated Sequences of COX1, ND5, and CYTB

Haplotype network analysis based on concatenated sequences of Ae. albopictus identified two major groups: a mainland group and a southern coastal group (Figure S1). The mainland group was dominated by a central haplotype (Hc1) with several closely related satellite haplotypes (Hc2–Hc4 and Hc8–Hc10). The southern coastal group consisted mainly of haplotypes from Busan and southern Korea (Hc5, Hc6, and Hc11).
Haplotype Hc7 (Busan4, H41) linked the southern coastal group to Southeast Asian haplotypes from Thailand and the Philippines and was also connected to haplotypes from China, Japan, Italy, Portugal, Greece, and the United States. Overall, the concatenated network showed a pattern similar to that based on COX1 alone.

3.4. Phylogenetic and Genetic Distance

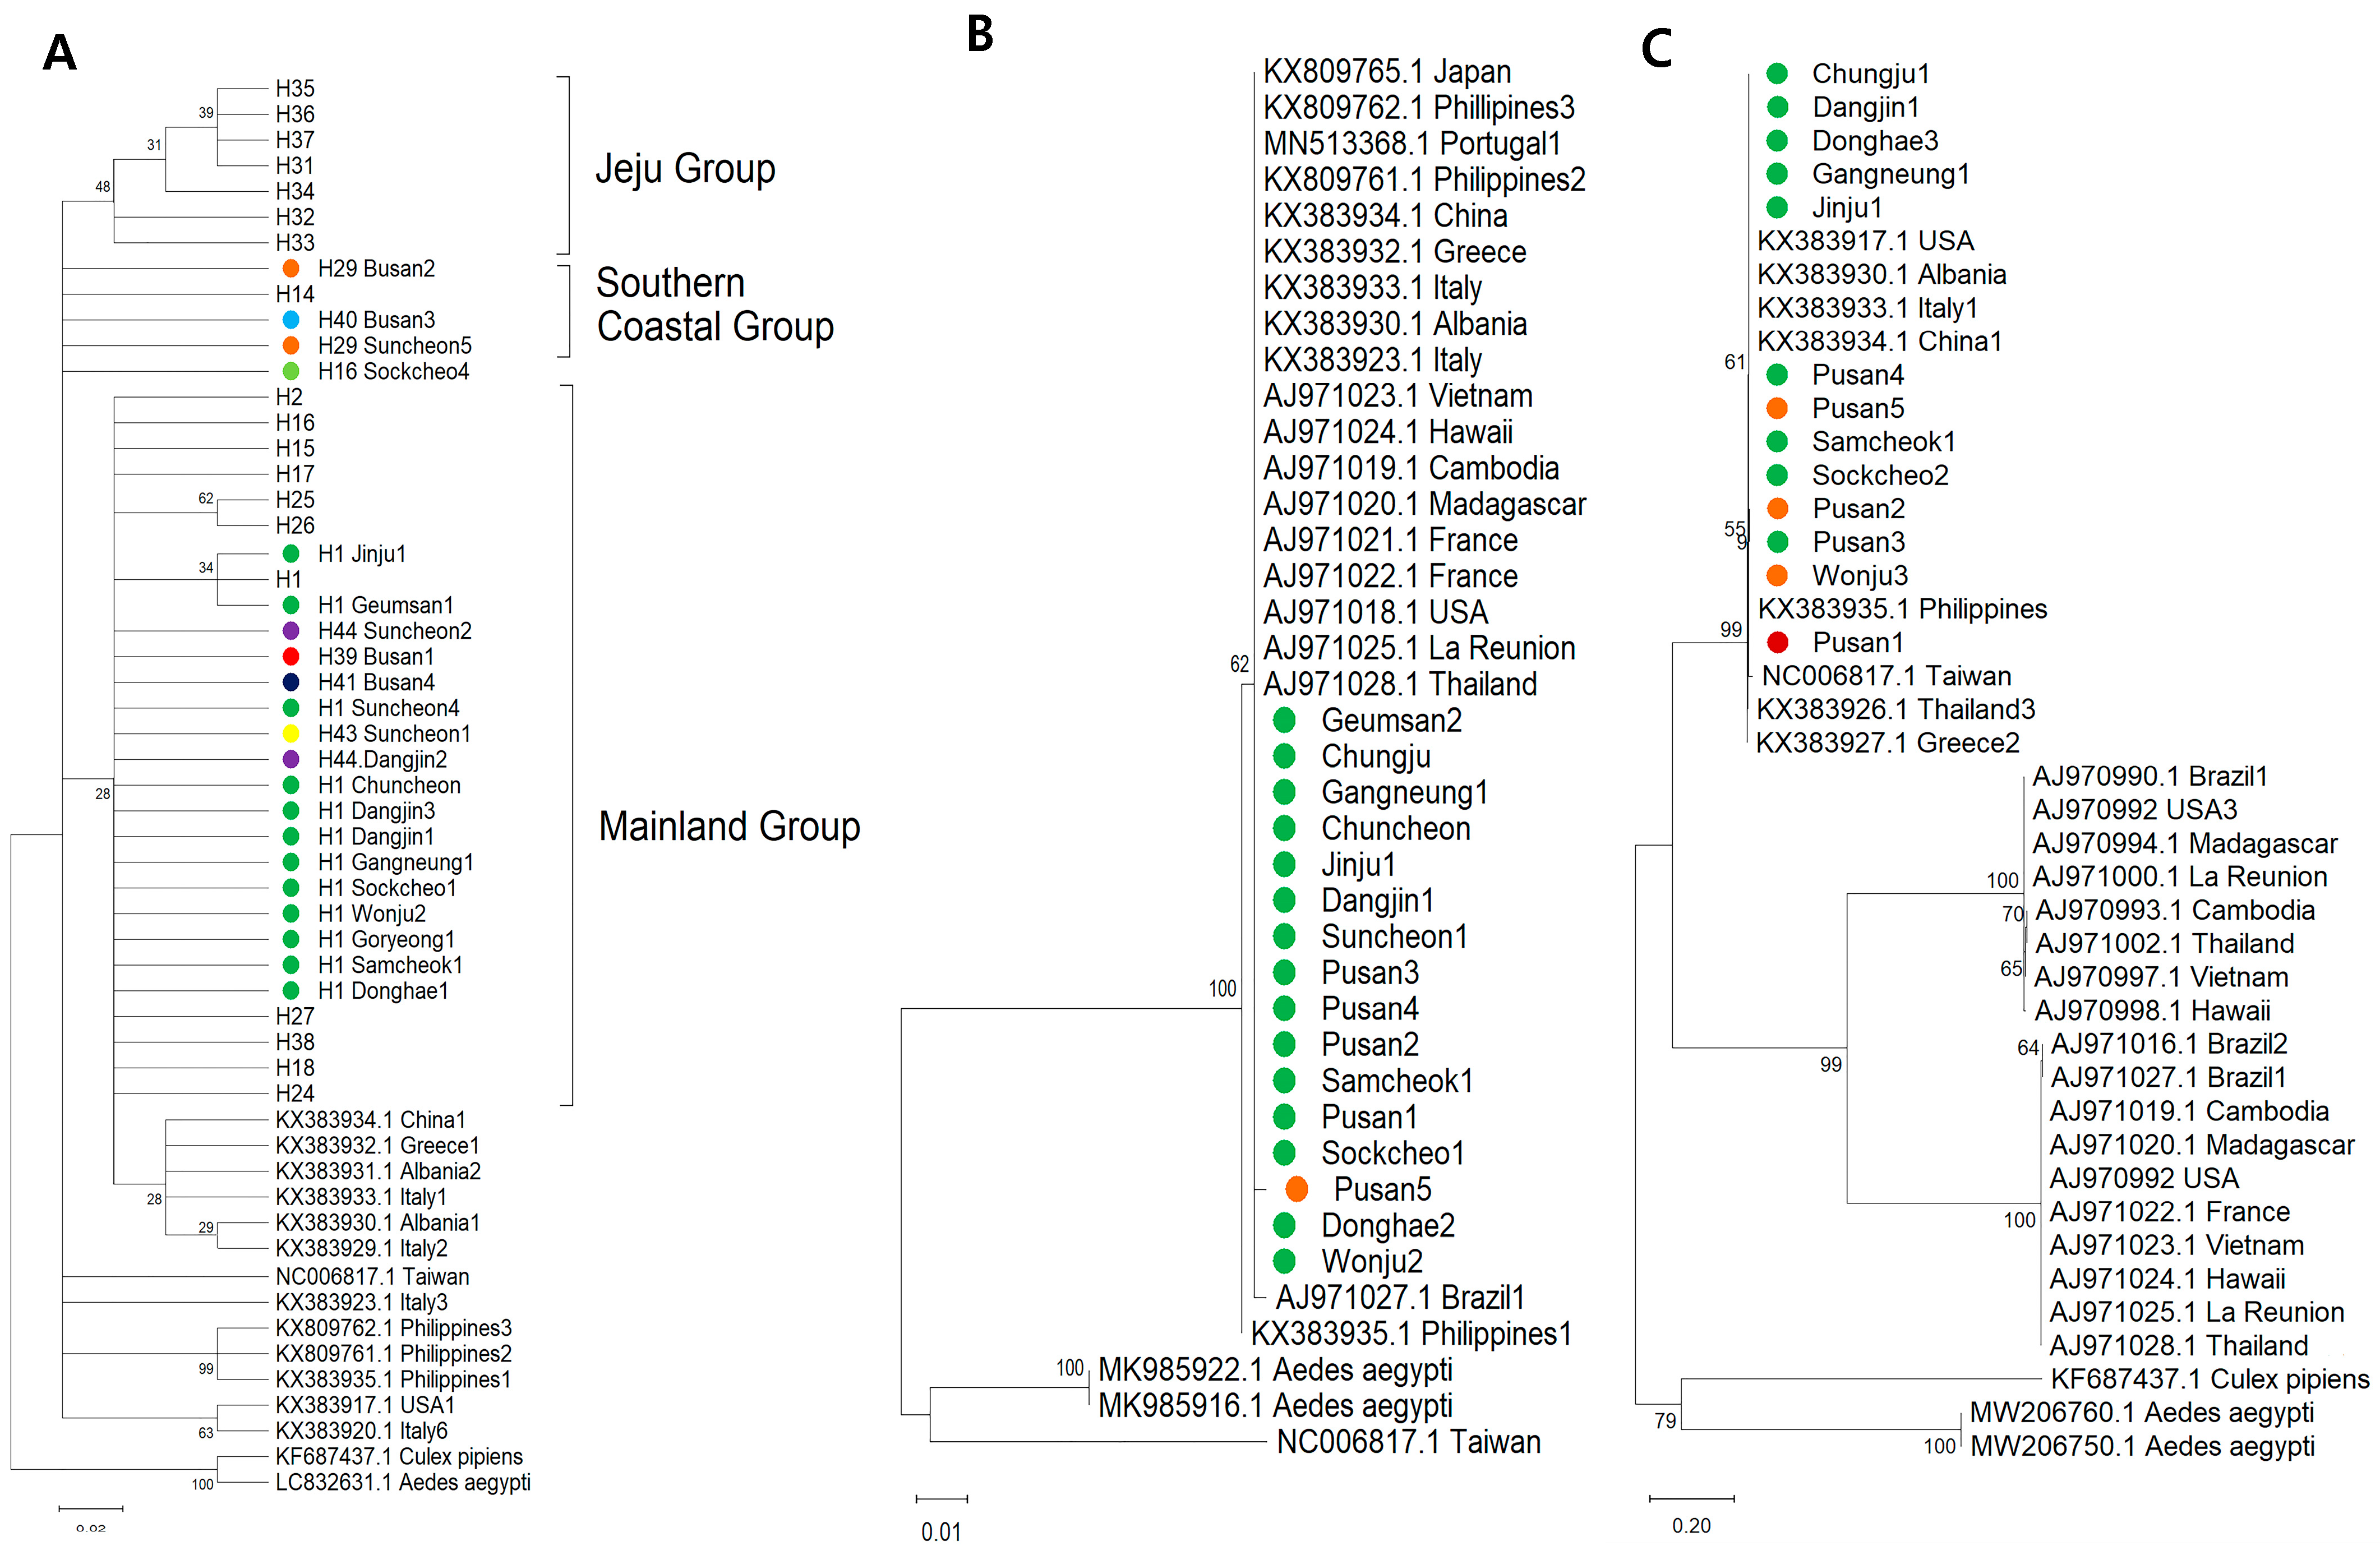
To examine the phylogenetic relationships of Ae. albopictus populations, phylogenetic trees were constructed using the maximum likelihood method. Sequences of three mitochondrial genes—COX1, ND5, and CYTB—from Aedes albopictus were aligned and analyzed alongside datasets obtained from GenBank. A total of 48 COX1 sequences, 46 ND5 sequences, and 47 CYTB sequences of Ae. albopictus from Korea were aligned with corresponding datasets retrieved from GenBank. (Figure 3).

3.4.1. Phylogenetic Analysis of Ae. albopictus Based on COX1

Phylogenetic analysis of COX1 sequences revealed three distinct clades of Ae. albopictus in Korea: the mainland, Jeju, and southern coastal groups (Figure 3A). The mainland group was distinct from those in China, Portugal, Brazil, Greece, and Albania. The Jeju group formed a clearly isolated cluster. The southern coastal group clustered near Thailand and Greece, but remained genetically distinct, showing no close relationship to geographically proximate Japan. The Philippines formed an independent and distinct cluster, with high support (bootstrap = 95).

3.4.2. Phylogenetic Analysis of Ae. albopictus Based on ND5 and CYTB

A phylogenetic tree of ND5 sequences showed that the predominant Korean haplotype (HND51) and HND52 from Busan clustered closely with Philippine haplotypes 1 and 4 and the BrazilianND5 haplotype, whereas Taiwan sequences were more distantly related—consistent with the ND5 haplotype network (Figure 3B).
For CYTB, two major clades were identified: one comprising sequences from Korea, along with international sequences from the Philippines, Thailand, China, Brazil, and Greece, Italy, Albania, and the USA (Figure 3C). This broad clustering indicates that the dominant Korean CYTB haplotypes are part of a widely distributed global mitochondrial lineage. The second major clade branched separately with high bootstrap support, indicating an evolutionarily distinct mitochondrial lineage.

3.4.3. Phylogenetic Analysis of Ae. albopictus Based on Concatenated Sequences of COX1, ND5, and CYTB

A phylogenetic tree based on concatenated sequences is divided into two major groups: the mainland group and the southern coastal group (Figure S2). The mainland population formed a relatively dense cluster consisting of haplotypes Hc1—Hc4 and Hc8—Hc10. In contrast, the southern coastal population included haplotypes Hc5, Hc6, and Hc11, which clustered with Southeast Asian and European haplotypes. Notably, Hc7 (Busan 4) was closely associated with overseas haplotypes, suggesting potential linkages between Korean and foreign populations. Overall, the phylogenetic patterns were consistent with the haplotype network analysis.

4. Discussion

In this study, we analyzed the phylogenetic diversity of the Asian tiger mosquito, Ae. albopictus in Korea using mitochondrial COX1, ND5, and CYTB markers, including analyses based on concatenated sequences. Our findings reveal important insights into the introduction pathways and regional dynamics of this globally invasive vector.
The COX1 marker of Ae. albopictus in Korea revealed various haplotypes, indicating that Korean Ae. albopictus population is genetically diverse rather than uniform [25,35]. COX1 analysis showed that southern coastal regions—particularly Busan and Suncheon—harbor the greatest haplotype diversity. This elevated diversity is a classic indicator of repeated introductions or ongoing gene flow from external sources [11]. Similar patterns have been observed in international port cities worldwide, where Aedes populations continually receive new lineages through trade and transportation [14]. Thus, the high diversity in Korea’s southern coastal regions likely reflects strong connectivity with foreign populations via maritime traffic [10,14]. In contrast, Jeju Island showed a distinct and isolated genetic cluster. Its differentiation mirrors patterns reported from geographically separated regions such as Malaysia, where local mosquito populations maintain unique genetic signatures despite potential dispersal [16]. This reinforces the idea that islands and ecologically isolated areas preserve region-specific lineages and may act as reservoirs of local diversity. ND5 and CYTB markers showed very limited diversity across Korea, possibly reflecting regional differences. Moreover, although these markers may be suitable for broad-scale diversity analyses, they appear less appropriate for fine-scale diversity assessments. Nonetheless, variation in CYTB sequences—similar to COX1—clearly characterized local diversification in the southern coastal region, and independent diversification was also found in the Wonju area. Analysis based on concatenated COX1, ND5, and CYTB sequences detected a larger number of haplotypes and higher haplotype diversity than analyses relying on COX1 alone, indicating improved genetic resolution. This suggests that integrating multiple mitochondrial loci captures a broader spectrum of intraspecific variation that may be overlooked by single-marker approaches. Importantly, the concatenated analysis enabled a nationwide characterization of genetic variation in Ae. albopictus populations across Korea (Figure 1D), providing a more comprehensive view of population connectivity and regional differentiation.
A key finding of this study is the identification of the H41 haplotype from Busan, which acts as a genetic bridge connecting all three domestic population groups. H41 also shows close relationships with lineages from China, Japan, and parts of Southeast Asia. The presence of such a “bridge haplotype” is biologically meaningful: it suggests that certain lineages may repeatedly enter Korea via major ports, subsequently dispersing domestically and linking otherwise distinct populations. This finding highlights Busan’s pivotal role as a national gateway for mosquito dispersal. Similar patterns have been documented in Europe, where highways, ports, and trade routes drive the rapid redistribution of Aedes mosquitoes across distant regions [11,13,14]. Phylogenetic analyses validated the three domestic groups and confirmed the intermediate, connector-like role of the Busan H41 haplotype among both Korean and foreign lineages. Together, these results reinforce the hypothesis that southern coastal Korea is experiencing continuous mosquito introductions, potentially influenced by increasing global trade, warming climates, and expanding mosquito habitat suitability [13].
Importantly, the identification of Busan as a genetic gateway has direct implications for vector surveillance strategies. Enhanced and sustained monitoring at international ports, cargo terminals, and surrounding urban areas should be prioritized to detect newly introduced lineages at an early stage. In contrast, the genetic distinctness of Jeju Island suggests limited gene flow with mainland populations, indicating that the island’s population may follow independent evolutionary and epidemiological trajectories. Therefore, Jeju Island should be monitored through separate, region-specific surveillance programs.
The broader implications of these findings are substantial. First, the strong genetic structuring in Korea suggests that Ae. albopictus populations are shaped by both natural geographic constraints and human-mediated movement. Second, the presence of genetically diverse lineages in port cities highlights the ongoing risk of introducing foreign vector populations—including those potentially carrying exotic arboviruses. Finally, the observed patterns align with global invasion models predicting the continued expansion of Ae. albopictus into new regions under climate change scenarios.
Collectively, our results emphasize the need for strengthened mosquito surveillance in coastal regions, targeted monitoring of introduction pathways, and integrated vector management strategies that account for both domestic population structure and international connectivity.
While mitochondrial COX1 remains a useful marker for species identification and broad phylogeographic comparisons in Aedes mosquitoes, its limited variability restricts its ability to resolve fine-scale population structure. In the present study, analyses based on concatenated COX1, ND5, and CYTB sequences partially overcome this limitation by detecting a greater number of haplotypes and higher haplotype diversity than COX1 alone. The concatenated approach enabled a more comprehensive assessment of nationwide genetic variation.
Nevertheless, mitochondrial markers represent a single, maternally inherited genome and therefore provide limited insight into complex demographic processes. In contrast, genome-wide SNPs, derived from thousands of nuclear loci, provide substantially higher resolution. Therefore, future detailed analyses of gene flow, population history, and microgeographic differentiation will benefit from the application of genome-wide SNP approaches [36].

5. Conclusions

In conclusion, this study highlights the complex phylogeographic structure and genetic diversity of Ae. albopictus in Korea. Analyses of COX1, ND5, and CYTB sequences revealed that southern coastal regions, particularly Busan, harbor the highest genetic diversity, likely reflecting repeated introductions and gene flow from foreign populations. Jeju Island populations formed a distinct cluster, emphasizing the influence of geographic isolation on local genetic structure. The identification of a “bridge haplotype” in Busan underscores the role of major ports in connecting domestic and international mosquito populations, facilitating both regional dispersal and potential long-distance introductions. These findings have direct implications for vector surveillance. As a genetic gateway, Busan and other major port cities should be prioritized for port-based inspections, early detection of introduced lineages, and targeted control. In contrast, the genetic distinctness of Jeju Island warrants separate, region-specific monitoring to track local population dynamics and prevent external introductions. Overall, southern coastal regions emerge as key entry points for Ae. albopictus, underscoring the need for enhanced surveillance, targeted vector management to mitigate the public health risks posed by this invasive mosquito species.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/insects17010082/s1, Table S1. Collection sites and collection of Aedes albopictus in Korea; Table S2. Primer sequences used for amplification of mitochondrial genes in Aedes albopictus; Table S3. Pairwise genetic distances of the haplotype of Aedes albopictus populations based on COX1 sequences in Korea and other regions; Table S4. Pairwise genetic distances of the haplotype of Aedes albopictus populations based on ND5 sequences in Korea and other regions; Table S5. Pairwise genetic distances of the haplotype of Aedes albopictus populations based on CYTB sequences in Korea and other regions; Table S6. Pairwise genetic distances of the haplotype of Aedes albopictus populations based on the concatenated sequence of COX1, ND5, and CYTB in Korea and other regions. Figure S1. Haplotype network of Aedes albopictus based on concatenated sequences of COX1, ND5, and CYTB from Korea and data set obtained from other regions. Core haplotypes are highlighted in yellow; Figure S2. Phylogenetic trees of Aedes albopictus based on concatenated sequences of COX1, ND5, and CYTB. Phylogenetic analyses were conducted using the maximum-likelihood (ML) method based on the sequences obtained in this study and data set retrieved from GenBank.

Author Contributions

Conceptualization, J.-U.J., I.-Y.L. and B.-Y.J.; methodology, S.M., I.T., I.-Y.L. and H.J.; software, J.-U.J. and S.M.; validation, I.T., H.J. and J.-H.H.; formal analysis, J.-U.J., I.T., H.J. and J.-H.H.; investigation, S.L. and I.T.; resources, J.-H.H. and F.M.; data curation, S.L., I.-Y.L. and F.M.; writing—original draft preparation, J.-U.J. and S.M.; writing—review and editing, I.-Y.L., F.M. and B.-Y.J.; visualization, J.-U.J., S.M. and S.L.; supervision, J.-H.H., F.M., K.-J.L. and B.-Y.J.; project administration, K.-J.L. and B.-Y.J.; funding acquisition, K.-J.L., and B.-Y.J. All authors have read and agreed to the published version of the manuscript.

Funding

This study was supported by the Institute for Basic Science (IBS), Republic of Korea (project code IBS-R801-D1-2025-A01), the National Institute of Health Research Project (Project No. 2024-ER2111-00 and 2022-NI-034), and the Climate Change Vector Surveillance Program of the Korea Disease Control and Prevention Agency (KDCA).

Data Availability Statement

The original data used for the analyses can be obtained from the authors after approval by the responsible initiations in Korea.

Acknowledgments

We would like to express our gratitude to the researchers at the Korea Disease Control and Prevention Agency (KDCA) for their valuable advice and support in mosquito collection and classification.

Conflicts of Interest

Author Sezim Monoldorova was employed by the company One Health Frontiers. The remaining authors declare that the research was conducted in the absence of any commercial or financial relationships that could be construed as a potential conflict of interest.

Appendix A

Table A1. GenBank accession numbers of the COX1 sequences of Ae. albopictus in this study.
Locality NameGeneGenBank Accession Number
Donghae_1COX1PX529948PX518777
Donghae_2COX1PX529949PX518778
Donghae_3COX1PX529950PX518779
Donghae_5COX1PX529951PX518780
Donghae_6COX1PX529952PX518781
Donghae_7COX1PX529953PX518782
Sockcheo_1COX1PX529954PX518783
Sockcheo_2COX1PX529955PX518784
Sockcheo_3COX1PX529956PX518785
Sockcheo_4COX1PX529957PX518786
Gangneung_1COX1PX529967PX518797
ChuncheonCOX1PX529976PX518806
Samcheok_1COX1PX529958PX518787
Samcheok_2COX1PX529959PX518788
Samcheok_3COX1PX529960PX518789
Samcheok_4COX1PX529961PX518790
Wonju_2COX1PX529962PX518792
Wonju_3COX1PX529963PX518793
Wonju_4COX1PX529964PX518794
Wonju_5COX1PX529965PX518795
Wonju_6COX1PX529966PX518796
Dangjin_1COX1PX529971PX518801
Dangjin_2COX1PX529972PX518802
Dangjin_3COX1PX529973PX518803
Dangjin_4COX1PX529974PX518804
Dangjin_5COX1PX529975PX518805
Geumsan_1COX1 PX518818
Geumsan_2COX1 PX518819
Geumsan_3COX1 PX518820
Geumsan_4COX1 PX518821
Geumsan_5COX1 PX518822
Suncheon_1COX1 PX518807
Suncheon_2COX1 PX518808
Suncheon_4COX1 PX518809
Suncheon_5COX1 PX518810
Goryeong_1COX1 PX518798
Goryeong_2COX1 PX518799
Goryeong_3COX1 PX518800
Jinju_1COX1 PX518815
Jinju_2COX1 PX518816
Jinju_3COX1 PX518817
Busan_1COX1 PX518811
Busan_2COX1 PX518812
Busan_3COX1 PX518813
Busan_4COX1 PX518814
Table A2. GenBank accession numbers of the ND5 and CYTB sequences of Ae. albopictus in this study.
Locality NameGenBank Accession Number
ND5CYTB
Donghae_2PX511435PX511394
Donghae_3PX511436PX511395
Donghae_5PX511437PX511397
Donghae_6PX511438PX511398
Donghae_7PX511439
Sockcheo_2 PX511399
Sockcheo_3PX511441PX511400
Sockcheo_4PX511442
Gangneung_1PX511443PX511401
Gangneung_2 PX511444
ChuncheonPX511450PX511402
Samcheok_1PX511431PX511389
Samcheok_2PX511432PX511390
Samcheok_3PX511433PX511391
Samcheok_4PX511434PX511392
Samcheok_6 PX511393
Wonju_2PX511445PX511403
Wonju_3PX511446PX511404
Wonju_4PX511447PX511405
Wonju_5PX511448PX511406
Wonju_6PX511449PX511407
Chungju_1PX511451PX511408
Dangjin_1PX511452PX511409
Dangjin_2PX511453PX511410
Dangjin_3PX511454PX511411
Dangjin_4PX511455PX511412
Dangjin_5PX511456PX511413
Dangjin_7 PX511414
Geumsan_1PX511457PX511415
Geumsan_2PX511458PX511416
Geumsan_3PX511459PX511417
Geumsan_4PX511460PX511418
Geumsan_5PX511461
Suncheon_1PX511462PX511419
Suncheon_2PX511463PX511420
Suncheon_3PX511464PX511421
Suncheon_4PX511465
Suncheon_5PX511466
Goryeong_1 PX511422
Jinju_1PX511467PX511423
Jinju_2PX511468PX511424
Jinju_3PX511469PX511425
Busan_1PX511470PX511426
Busan_2PX511471PX511427
Busan_3PX511472PX511428
Busan_4PX511473PX511429
Busan_5PX511474PX511430

References

  1. Shuman, E.K. Global climate change and infectious diseases. N. Engl. J. Med. 2010, 362, 1061–1063. [Google Scholar] [CrossRef] [Scilit]
  2. Liu-Helmersson, J.; Brännström, Å.; Sewe, M.; Semenza, J.C.; Rocklöv, J. Estimating past, present, and future trends in the global distribution and abundance of the arbovirus vector Aedes aegypti under climate change scenarios. Front. Public Health 2019, 7, 148. [Google Scholar] [CrossRef] [Scilit]
  3. Pourzangiabadi, M.; Najafi, H.; Fallah, A.; Goudarzi, A.; Pouladi, I. Dengue virus: Etiology, epidemiology, pathobiology, and developments in diagnosis and control—A comprehensive review. Infect. Genet. Evol. 2025, 127, 105710. [Google Scholar] [CrossRef] [Scilit]
  4. Kori, M.; Awano, N.; Inomata, M.; Kuse, N.; Tone, M.; Yoshimura, H.; Jo, T.; Takada, K.; Tanaka, A.; Mawatari, M.; et al. The 2014 autochthonous dengue fever outbreak in Tokyo: A case series study and assessment of the causes and preventive measures. Respir. Med. Case Rep. 2020, 31, 101246. [Google Scholar] [CrossRef] [Scilit]
  5. Rezza, G.; Nicoletti, L.; Angelini, R.; Romi, R.; Finarelli, A.C.; Panning, M.; Cassone, A. Infection with chikungunya virus in Italy: An outbreak in a temperate region. Lancet 2007, 370, 1840–1846. [Google Scholar] [CrossRef] [Scilit]
  6. World Health Organization. Chikungunya: Fact Sheet. World Health Organization Website. April 2025. Available online: https://www.who.int/news-room/fact-sheets/detail/chikungunya (accessed on 1 October 2025).
  7. Kim, H.; Cha, G.W.; Jeong, Y.E.; Lee, W.G.; Chang, K.S.; Roh, J.Y.; Yang, S.C.; Park, M.Y.; Park, C.; Shin, E.H. Detection of Japanese encephalitis virus genotype V in Culex orientalis and Culex pipiens (Diptera: Culicidae) in Korea. PLoS ONE 2015, 10, e0116547. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Centers for Disease Control and Prevention (CDC). Aedes aegypti and Aedes albopictus—Mosquito Maps. CDC Website. 2024. Available online: https://www.cdc.gov/mosquitoes (accessed on 1 October 2025).
  9. Messina, J.P.; Brady, O.J.; Golding, N.; Kraemer, M.U.G.; Wint, G.R.W.; Ray, S.E.; Pigott, D.M.; Shearer, F.M.; Johnson, K.; Earl, L.; et al. The current and future global distribution and population at risk of dengue. Nat. Microbiol. 2019, 4, 1508–1515. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Kraemer, M.U.; Sinka, M.E.; Duda, K.A.; Mylne, A.Q.; Shearer, F.M.; Barker, C.M.; Moore, C.G.; Carvalho, R.G.; Coelho, G.E.; Van Bortel, W.; et al. The global distribution of the arbovirus vectors Aedes aegypti and Ae. albopictus. eLife 2015, 4, e08347. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Medlock, J.M.; Hansford, K.M.; Schaffner, F.; Versteirt, V.; Hendrickx, G.; Zeller, H.; Van Bortel, W. A review of the invasive mosquitoes in Europe: Ecology, public health risks, and control options. Vector Borne Zoonotic Dis. 2012, 12, 435–447. [Google Scholar] [CrossRef] [Scilit]
  12. Benedict, M.Q.; Levine, R.S.; Hawley, W.A.; Lounibos, L.P. Spread of the tiger: Global risk of invasion by the mosquito Aedes albopictus. Vector Borne Zoonotic Dis. 2007, 7, 76–85. [Google Scholar] [CrossRef] [Scilit]
  13. Eritja, R.; Palmer, J.R.; Roiz, D.; Sanpera-Calbet, I.; Bartumeus, F. Direct evidence of adult Aedes albopictus dispersal by car. Sci. Rep. 2016, 6, 38152. [Google Scholar] [CrossRef] [Scilit]
  14. Kraemer, M.U.G.; Reiner, R.C., Jr.; Brady, O.J.; Messina, J.P.; Gilbert, M.; Pigott, D.M.; Yi, D.; Johnson, K.; Earl, L.; Marczak, L.B.; et al. Past and future spread of the arbovirus vectors Aedes aegypti and Aedes albopictus. Nat. Microbiol. 2019, 4, 854–863. [Google Scholar] [CrossRef] [Scilit]
  15. Brown, W.M.; George, M., Jr.; Wilson, A.C. Rapid evolution of animal mitochondrial DNA. Proc. Natl. Acad. Sci. USA 1979, 76, 1967–1971. [Google Scholar] [CrossRef] [Scilit]
  16. Ismail, N.A.; Adilah-Amrannudin, N.; Hamsidi, M.; Ismail, R.; Dom, N.C.; Ahmad, A.H.; Mastuki, M.F.; Camalxaman, S.N. The genetic diversity, haplotype analysis, and phylogenetic relationship of Aedes albopictus (Diptera: Culicidae) based on the cytochrome oxidase 1 marker: A Malaysian scenario. J. Med. Entomol. 2017, 54, 1573–1581. [Google Scholar] [CrossRef] [Scilit]
  17. Mousson, L.; Dauga, C.; Garrigues, T.; Schaffner, F.; Vazeille, M.; Failloux, A.B. Phylogeography of Aedes (Stegomyia) aegypti (L.) and Aedes (Stegomyia) albopictus (Skuse) (Diptera: Culicidae) based on mitochondrial DNA variations. Genet. Res. 2005, 86, 1–11. [Google Scholar] [CrossRef] [Scilit]
  18. Adilah-Amrannudin, N.; Hamsidi, M.; Ismail, N.A.; Ismail, R.; Dom, N.C.; Ahmad, A.H.; Mastuki, M.F.; Basri, T.S.; Khalid, A.; Muslim, M.; et al. Genetic polymorphism of Aedes albopictus population inferred from ND5 gene variabilities in Subang Jaya, Malaysia. J. Am. Mosq. Control Assoc. 2016, 32, 265–272. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Usmani-Brown, S.; Cohnstaedt, L.; Munstermann, L.E. Population Genetics of Aedes albopictus (Diptera: Culicidae) invading populations, using mitochondrial Nicotinamide Adenine Dinucleotide Dehydrogenase Subunit 5 Sequences. Ann. Entomol. Soc. Am. 2009, 102, 144–150. [Google Scholar] [CrossRef] [Scilit]
  20. Palacio-Cortés, A.M.; Valencia-Marin, B.S.; Navarro-Silva, M.A. Exploring the genetic variability and population structure of Aedes albopictus Populations in Southeast Brazil. Acta Parasitol. 2025, 70, 187. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Seddigh, S.; Darabi, M. Functional, structural, and phylogenetic analysis of mitochondrial cytochrome b (cytb) in insects. Mitochondrial DNA A DNA Mapp Seq Anal. 2018, 29, 236–249. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Krzywinski, J.; Wilkerson, R.C.; Besansky, N.J. Toward understanding Anophelinae (Diptera, Culicidae) phylogeny: Insights from nuclear single-copy genes and the weight of evidence. Syst. Biol. 2001, 50, 540–556. [Google Scholar] [CrossRef]
  23. Pech-May, A.; Moo-Llanes, D.A.; Puerto-Avila, M.B.; Casas, M.; Danis-Lozano, R.; Ponce, G.; Tun-Ku, E.; Pinto-Castillo, J.F.; Villegas, A.; Ibáñez-Piñon, C.R.; et al. Population genetics and ecological niche of invasive Aedes albopictus in Mexico. Acta Trop. 2016, 157, 30–41. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Lee, S.H.; Nam, K.W.; Jeong, J.Y.; Yoo, S.J.; Koh, Y.S.; Lee, S.; Heo, S.T.; Seong, S.Y.; Lee, K.H. The effects of climate change and globalization on mosquito vectors: Evidence from Jeju Island, South Korea on the potential for Asian tiger mosquito (Aedes albopictus) influxes and survival from Vietnam rather than Japan. PLoS ONE 2013, 8, e68512. [Google Scholar] [CrossRef] [Scilit]
  25. Shin, J.; Jung, J. Comparative population genetics of the invasive mosquito Aedes albopictus and the native mosquito Aedes flavopictus in the Korean peninsula. Parasites Vectors 2021, 14, 377. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Ree, H.I. Taxonomic review and revised keys of the Korean mosquitoes (Diptera: Culicidae). Korean J. Entomol. 2003, 33, 39–52. [Google Scholar] [CrossRef] [Scilit]
  27. Folmer, O.; Black, M.; Hoeh, W.; Lutz, R.; Vrijenhoek, R. DNA primers for amplification of mitochondrial cytochrome c oxidase subunit I from diverse metazoan invertebrates. Mol. Mar. Biol. Biotechnol. 1994, 3, 294–299. [Google Scholar]
  28. Birungi, J.; Munstermann, L.E. Genetic structure of Aedes albopictus (Diptera: Culicidae) populations based on mitochondrial ND5 sequences: Evidence for an independent invasion into Brazil and United States. Ann. Entomol. Soc. Am. 2002, 95, 125–132. [Google Scholar] [CrossRef] [Scilit]
  29. Edgar, R.C. MUSCLE: Multiple sequence alignment with high accuracy and high throughput. Nucleic Acids Res. 2004, 32, 1792–1797. [Google Scholar] [CrossRef] [Scilit]
  30. Tamura, K.; Stecher, G.; Kumar, S. Molecular Evolutionary Genetics Analysis Version 11. Mol. Biol. Evol. 2021, 38, 3022–3027. [Google Scholar] [CrossRef] [Scilit]
  31. Needleman, S.B.; Wunsch, C.D. A general method applicable to the search for similarities in the amino acid sequence of two proteins. J. Mol. Biol. 1970, 48, 443–453. [Google Scholar] [CrossRef] [Scilit]
  32. Smith, T.F.; Waterman, M.S. Identification of common molecular subsequences. J. Mol. Biol. 1981, 147, 195–197. [Google Scholar] [CrossRef] [Scilit]
  33. Rozas, J.; Ferrer-Mata, A.; Sánchez-DelBarrio, J.C.; Guirao-Rico, S.; Librado, P.; Ramos-Onsins, S.E.; Sánchez-Gracia, A. DnaSP 6: DNA sequence polymorphism analysis of large data sets. Mol. Biol. Evol. 2017, 34, 3299–3302. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Leigh, J.W.; Bryant, D. POPART: Full-feature software for haplotype network construction. Methods Ecol. Evol. 2015, 6, 1110–1116. [Google Scholar] [CrossRef] [Scilit]
  35. Lee, E.; Yang, S.C.; Kim, T.K.; Noh, B.E.; Lee, H.S.; Kim, H.; Roh, J.Y.; Lee, W.G. Geographical genetic variation and sources of Korean Aedes albopictus (Diptera: Culicidae) populations. J. Med. Entomol. 2020, 57, 1057–1068. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Rašić, G.; Filipović, I.; Weeks, A.R.; Hoffmann, A.A. Genome-wide SNPs lead to strong signals of geographic structure and relatedness patterns in the major arbovirus vector, Aedes aegypti. BMC Genom. 2014, 15, 275. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Geographic distribution of Aedes albopictus haplotypes in South Korea. A total of 4658 mosquitoes were collected from 13 sites across seven provinces, of which 542 Ae. albopictus were analyzed. Mitochondrial haplotypes were determined based on analyses of (A) COX1, (B) ND5, (C) CYTB, and (D) concatenated sequences. The relative proportions of haplotypes at each collection site are shown as pie charts. Colors corresponded to distinct haplotypes, highlighting regional variation in genetic diversity.
Insects 17 00082 g001
Figure 2. Haplotype network of Aedes albopictus COX1 (A), ND5 (B), and CYTB (C) sequences from Korea and datasets obtained from other regions, which include haplotypes from the Korean Disease Control and Prevention Agency (KDCA) and GenBank. Core haplotypes are highlighted in yellow.
Insects 17 00082 g002
Figure 3. Phylogenetic trees of Aedes albopictus based on mitochondrial COX1 (A), ND5 (B), and CYTB (C) gene sequences. Phylogenetic analyses were conducted using the maximum-likelihood (ML) method based on the sequences obtained in this study and the dataset retrieved from GenBank. HND51 and HCYTB1 are shown in green, HND52 and HCYTB2 in orange, and HCYTB3 in red. HND51 and HND52 represent haplotypes based on the ND5 sequence of Ae. albopictus, whereas HCYTB1, HCYTB2, and HCYTB3 represent haplotypes based on the CYTB sequence of Ae. albopictus. The GenBank accession numbers for the Ae. albopictus COX1 sequences used in this study are provided in Table A1, while those for the ND5 and CYTB sequences are listed in Table A2.
Insects 17 00082 g003
Table 1. Haplotype and genetic diversity indices of Aedes albopictus populations based on COX1 sequences in Korea.
ProvinceLocalityNHHaplotypesHdπκS
GangwonSamcheok51H10.20470.00040.2111
Donghae61H1
Sockcheo32H1, H16
Gangneung11H1
Wonju61H1
Chuncheon11H1
ChungbukChungju21H10.3330.00030.3331
ChungnamDangjin52H1, H44
Geumsan51H1
JeonamSuncheon54H1, H29, H43, H440.3630.00030.4688
GyeongbukGoryeong11H1
GyeongnamJinju31H1
Busan Metropolitan55H29, H39, H40, H41, H42
Total489H1, H16, H29, H39~H440.3410.00050.6808
COX1, cytochrome c oxidase subunit 1; N, number of sequences; H, haplotype diversity; π, nucleotide diversity; κ, Average number of nucleotide differences; S, number of polymorphic sites. Hd, π, κ, and S were grouped by region—northeastern, central, and southern—and analyzed accordingly.
Table 2. Haplotype and genetic diversity indices of Aedes albopictus populations based on ND5 sequences in Korea.
ProvinceLocalityNHHaplotypesHdπκS
GangwonSamcheok51HND510
Donghae51HND51
Sockcheo31HND51
Gangneung11HND51
Wonju51HND51
Chuncheon11HND51
ChungbukChungju21HND510
ChungnamDangjin51HND51
Geumsan51HND51
JeonamSuncheon51HND510.1110.2910.1111
GyeongbukGoryeong11HND51
GyeongnamJinju31HND51
Busan Metropolitan52HND51, HND52
Total462HND51, HND520.0430.00010.0431
ND5, NADH dehydrogenase 5; N, number of sequences; H, haplotype diversity; π, nucleotide diversity; κ, Average number of nucleotide differences; S, number of polymorphic sites. Hd, π, κ, and S were grouped by region—northeastern, central, and southern—and analyzed accordingly.
Table 3. Haplotype and genetic diversity indices of Aedes albopictus populations based on CYTB sequences in Korea.
ProvinceLocalityNHHaplotypesHdπκS
GangwonSamcheok61HCYTB10.1820.00090.3410
Donghae61HCYTB1
Sockcheo31HCYTB1
Gangneung11HCYTB1
Wonju52HCYTB1, HCYTB2
Chuncheon11HCYTB1
ChungbukChungju21HCYTB10
ChungnamDangjin51HCYTB1
Geumsan51HCYTB1
JeonamSuncheon51HCYTB10.2220.00100.2222
GyeongbukGoryeong11HCYTB1
GyeongnamJinju31HCYTB1
Busan Metropolitan53HCYTB1, HCYTB2, HCYTB3
Total473HCYTB1, HCYTB2, HCYTB30.01620.00040.1652
CYTB; cytochrome b, N; number of sequences, H; haplotype diversity, π; nucleotide diversity, κ; Average number of nucleotide differences, S; number of polymorphic sites. Hd, π, κ, and S were grouped by region—northeastern, central, and southern—and analyzed accordingly.
Table 4. Haplotype and genetic diversity indices of Aedes albopictus populations based on concatenated sequences of COX1, ND5, and CYTB in Korea.
ProvinceLocalityNHHaplotypesHdπκS
GangwonSamcheok51Hc10.3480.00020.3713
Donghae51Hc1
Sockcheo32Hc1, Hc2
Gangneung11Hc1
Wonju52Hc1, Hc3
Chuncheon11Hc1
ChungbukChungju21Hc10.1670.00010.2002
ChungnamDangjin52Hc1, Hc10
Geumsan51Hc1
JeonamSuncheon54Hc1, Hc9, Hc10, Hc110.5710.00040.8769
GyeongbukGoryeong11Hc1
GyeongnamJinju31Hc1
Busan Metropolitan55Hc4, Hc5, Hc6, Hc7, Hc8
Total4611Hc1, Hc2, Hc3, Hc4, Hc5, Hc6, Hc7, Hc8, Hc9, Hc10, Hc11 0.4240.00040.92011
COX1, cytochrome c oxidase subunit 1; ND5, NADH dehydrogenase 5; CYTB, cytochrome b; N, number of sequences; H, haplotype diversity; π, nucleotide diversity; κ, Average number of nucleotide differences; S, number of polymorphic sites. Hd, π, κ, and S were grouped by region—northeastern, central, and southern—and analyzed accordingly.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.