


Abstract
Spherical distributions, in particular, the von Mises–Fisher distribution, are often used to analyze directional data. The first and second moments of these distributions are of central interest, as they describe mean orientations as well as anisotropic diffusion tensors. Finding these moments often requires a numerical approximation of complex trigonometric integrals. Instead, we apply the divergence theorem on suitable domains to derive explicit forms of the first and second moments for n-dimensional von Mises–Fisher and peanut distributions. Based on these new formulas, we characterize some meaningful characteristics of these distributions: fractional anisotropy and the anisotropy ratio. We find, surprisingly, that the peanut distribution has an upper bound on anisotropy, while the von-Mises Fisher distribution has no such bound. As a side benefit, we find different forms of some identities for Bessel functions.
Keywords:
spherical distributions; second moment; von Mises-Fisher distribution; peanut distribution; fractional anisotropy MSC:
92B15; 60E05; 62H11
1. Introduction
Spherical distributions are of special importance when working with directional data [1]. They are used to represent orientation of objects or individuals and identify movement directions. Recently, spherical distributions have been particularly important in the modelling of directed motion in biology. Examples in ecology that have been modelled include the directed motion of wolves along seismic lines [2], the orientation of sea turtles along geomagnetic lines [3], hilltopping of butterflies [4], and migration of whales [5]. Examples of directed cell movement include the movement of melanoma cells [6], spread of glioma in the brain [7], oriented motion of cells on microfabricated structures [8], and directed motion of immune cells [9].
Mathematically, a spherical distribution is a probability distribution on the unit sphere in , where denotes the space dimension. We usually denote it as , with the basic properties
For application to glioma, three spherical distributions have been proposed (we give explicit definitions later): the von Mises distribution (5) (also called von Mises–Fisher for higher dimensions), the peanut distribution (6), and the ordinary distribution function (ODF) (7) [7,10,11,12]. The von Mises distribution has been used in a model that was fit to data for 10 patients diagnosed with glioma in [7], while the ODF has been used for a theoretical model for glioma growth incorporating the effect from endothelial cells as well as the acidity from the environment in [12]. Here, we focus on the peanut and von Mises distributions. We generalize the distributions to any space dimensions and we compute new formulas for the expectation and variance–covariance matrices for these distributions. We also applied the method to the ODF distribution, but, unfortunately, we did not obtain an explicit formula for the second moment of the ODF distribution. Other important spherical distributions are the Bingham, the Fisher–Bingham, and the Kent distributions. These have not been used extensively in biological modelling; hence, we discuss them only briefly in the conclusion section.
1.1. Anisotropic Transport Equations
The popular use of spherical distributions in ecology and cell biology relies on the modelling of movement data with transport equations. In this short subsection, we recall some of the essential steps of this framework, to set the stage for the following calculations. Among the above applications, let us choose the example of wolf movement along seismic lines. The arguments for the other applications (glioma, immune cells, sea turtles, whales) are very similar.
Seismic lines are clear-cut lines in the Northern Canadian forests, which are cut by oil exploration companies to search for oil and gas [13]. Wolves in these forests can use these lines to migrate further than normal and increase their hunting success. Needless to say, this has a severe ecological impact. Using GPS data on wolf movement, it was shown by McKenzie et al. [2,14] that the directional orientation of wolves near seismic lines follows a von Mises distribution. Let us call it , .
To formulate a mathematical model for the wolf movement, we introduce a wolf density that depends on time t, location x, and orientation and consider the anisotropic transport equation
Here is a rate of change of direction and s is an average speed. The arguments of have been suppressed in three of the terms.
The analysis of these types of models is well established, many papers are available [15,16,17] and we will not recall any details here. However, we will discuss the important parabolic scaling. Parabolic scaling is a scaling transformation of the transport Equation (2) into macroscopic time and space scales. It can be shown that, to leading order the integrated particle density
satisfies an advection diffusion equation
where the drift velocity and the diffusion coefficient are proportional to the first and second moments of :
Hence, very clearly, knowledge of the first and second moments of is essential here.
In the application to wolf data, the distribution encodes the directional network of seismic lines in the environment [2,14]. In the case of sea turtles, describes the orientation towards the target site [3]. Applied to glioma data, is informed from an MRI imaging technique called diffusion tensor imaging (DTI) [7,12,18,19,20] (see also Section 5 for a simplified example).
Hillen et al. [10] calculated the explicit forms of the expectation and the variance–covariance matrix for the von Mises–Fisher distribution in two and three dimensions. It appears that the use of the divergence theorem in suitable domains was the key to obtaining the explicit formulas for the moments of these distributions.
1.2. Outline of the Paper
Here, we extend that methodology to higher dimensions. The advantage of knowing the explicit form of the moments for spherical distributions is that one can easily calculate the expectation and variance–covariance matrix without having to do the integrals numerically; hence, significantly reducing the computational cost for large dimensions. We find explicit forms for n-dimensional von Mises–Fisher and peanut distributions which, to our knowledge, are new formulas.
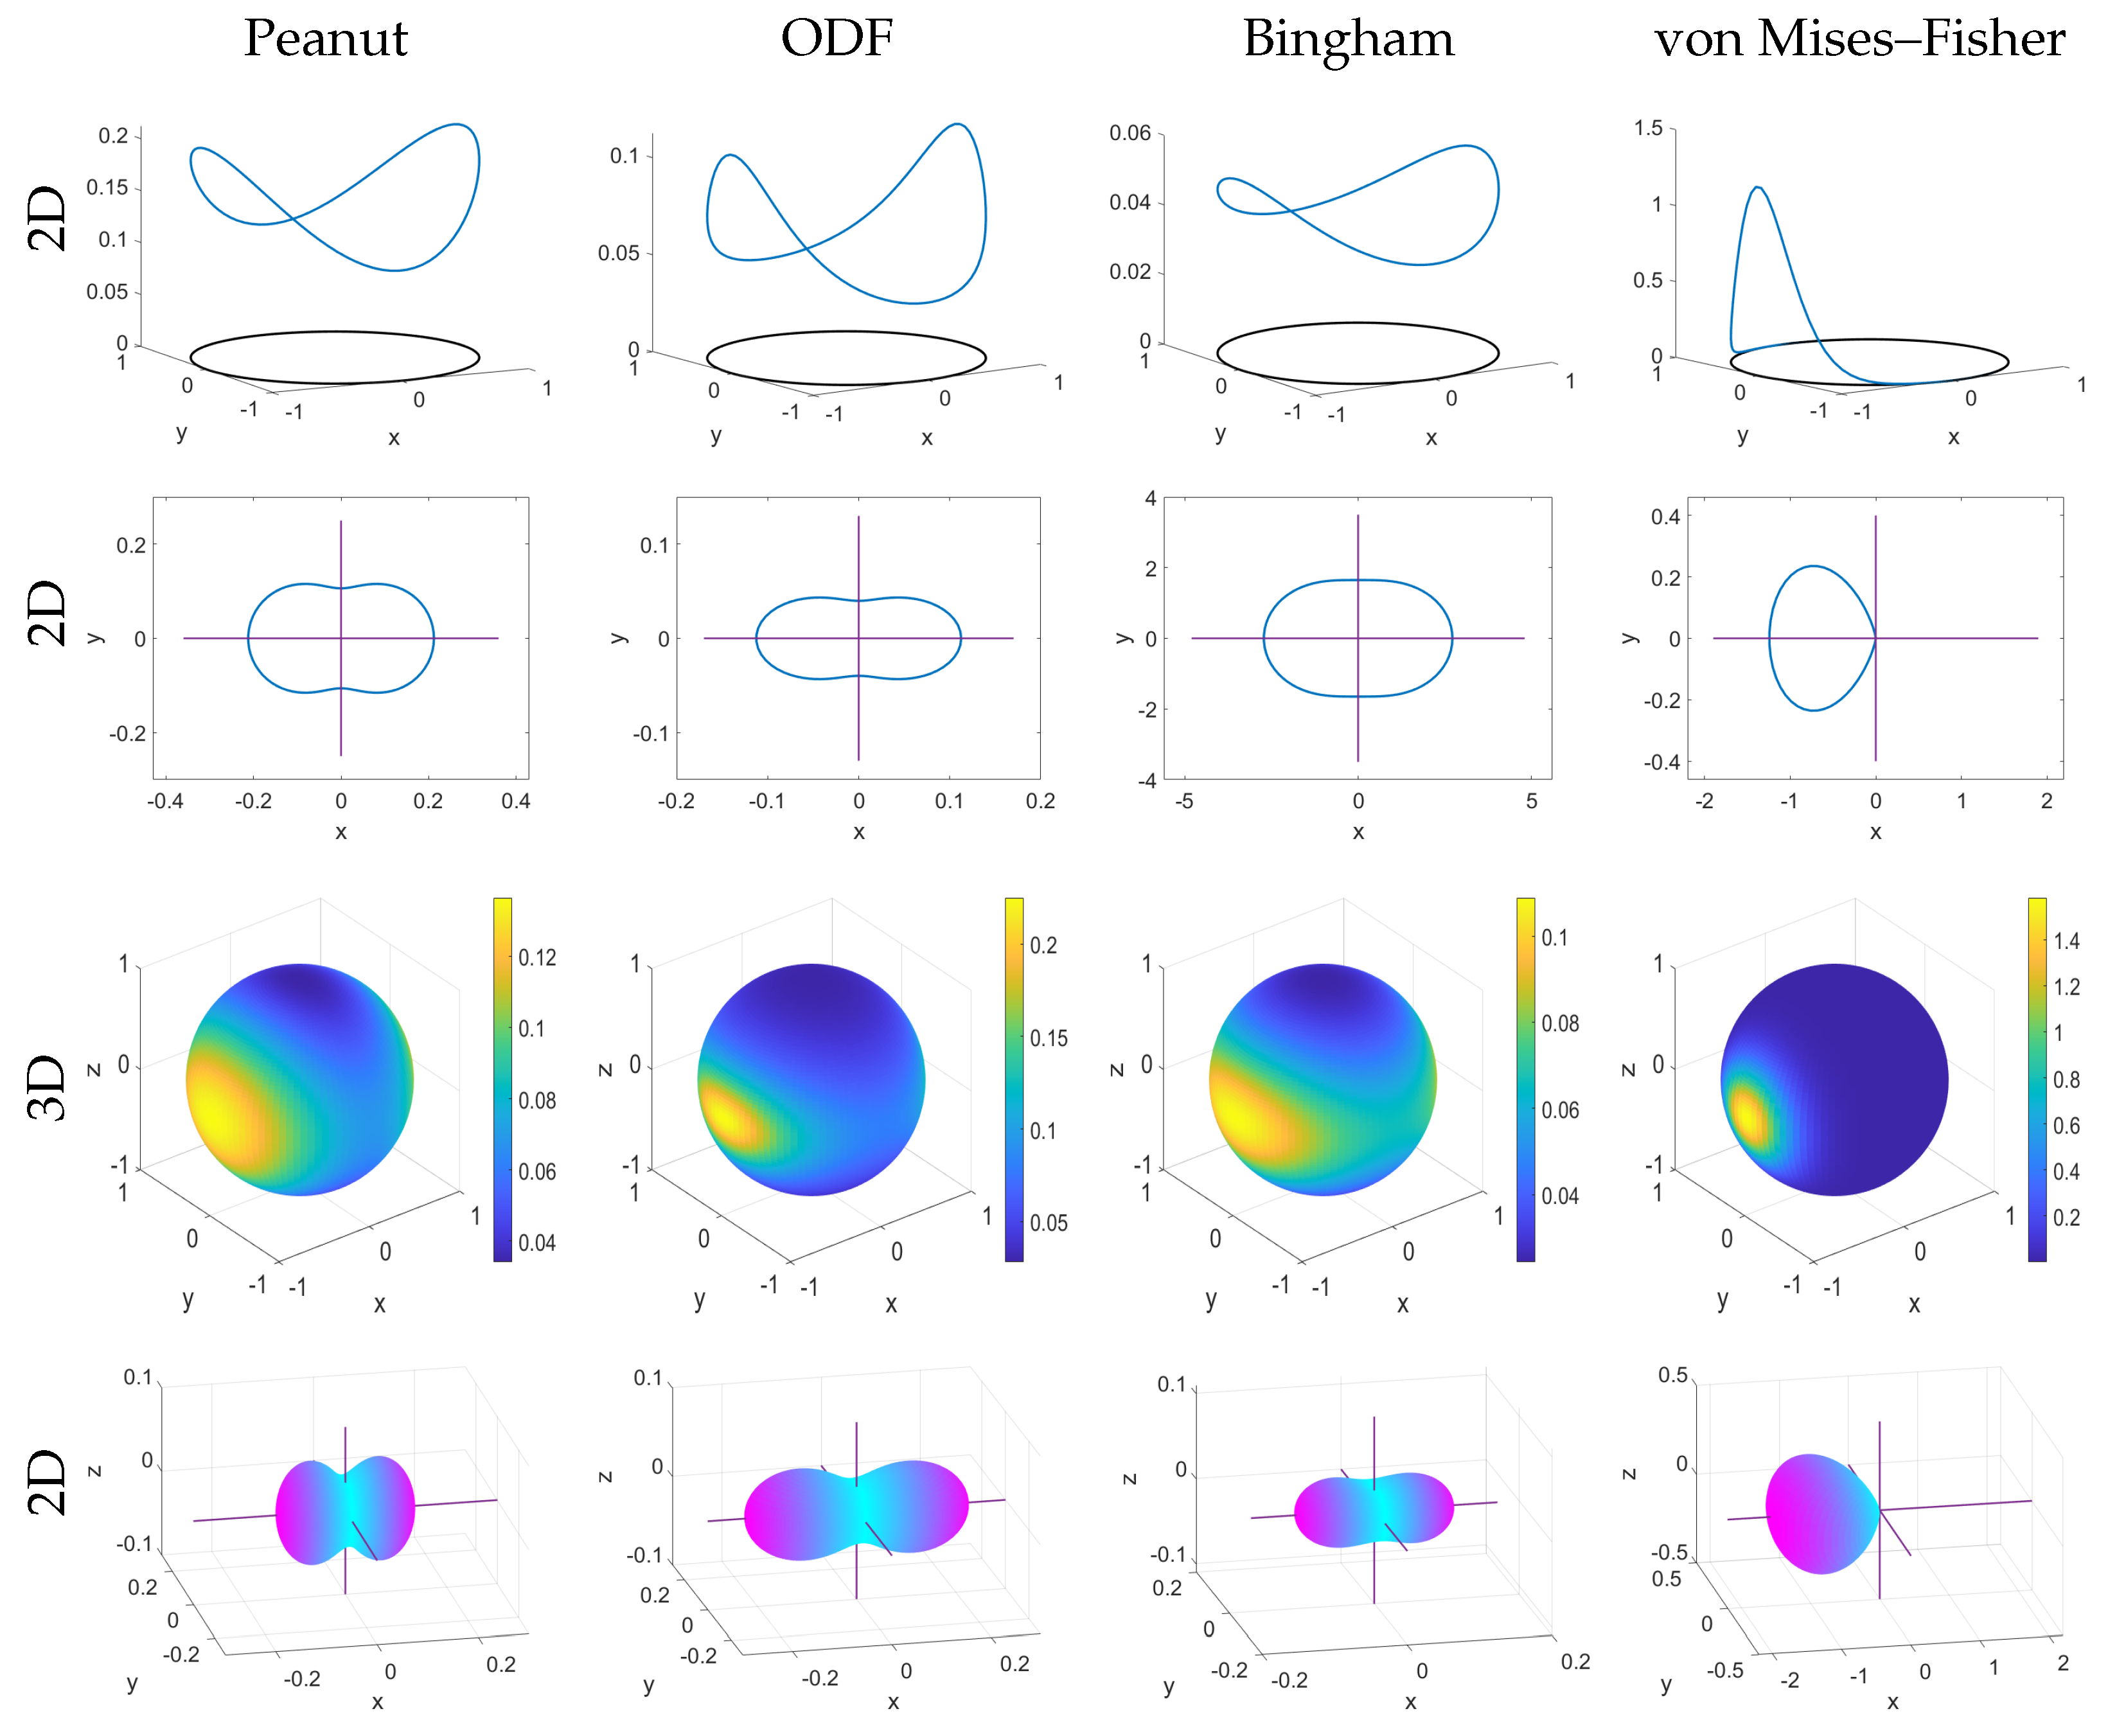
In addition, we consider the level of anisotropies that arise from these different formulations (peanut, ODF, von Mises–Fisher). The anisotropy is a measure of the distortion of the distribution in certain directions. It can be easily visualized by plotting level sets of the corresponding distributions (see Figure 1). To measure the anisotropy, we first compute the eigenvalues of the corresponding variance–covariance matrices, and then compute the fractional anisotropy () and the maximal eigenvalue ratio R. We find that peanut distribution has a limit to how much anisotropy it can account for, however the von Mises–Fisher does not have such a limitation, showing that the von Mises–Fisher is the better choice for capturing anisotropy. Please note that, here, we focus on theoretical results, specific applications are treated in the cited literature [2,3,7,14,17].
Figure 1.
Illustration of the spherical distributions in 2D and 3D (first and third rows, respectively) as well as their diffusion peanuts in 2D and 3D (second and last row, respectively). For the peanut, ODF, and Bingham distributions, was taken to be a diagonal matrix with , and on the main diagonal for 2D and 3D, respectively. For the Bingham distribution, . For von Mises–Fisher, and the preferred direction u was set to and for 2D and 3D, respectively. Note here that the peanut and ODF are symmetric (), whereas von Mises−Fisher is asymmetric.
1.3. Definitions of Some Spherical Distributions
In this section, we give the explicit definitions of the spherical distributions that we will work with. We use given parameters where is a concentration parameter, is a given vector, and is a given positive definite matrix. In the case of glioma modelling, A is estimated from the diffusion tensor data (see Section 5).
- The n-dimensional von Mises–Fisher distribution is defined as [10]where and with defines the modified Bessel function of the first kind of order p, k is the concentration parameter, and defines the likeliest direction of the distribution. Here, we employ a formulation that uses Bessel functions. An alternative definition uses the Gamma function and can be found in Appendix A.1.
- The n-dimensional peanut distribution is defined as [11]where denotes the trace of A, , and is the surface area of an dimensional sphere.
- The n-dimensional ODF distribution is defined as [12,21]where and A hold the same definitions as in the peanut distribution defined above. In (7), denotes the inverse of A and .
- We only briefly discuss the Bingham distribution [1,22], which is defined aswhere , A, hold the same definitions as above and is the diffusion time.
- The Fisher–Bingham distribution [1] is defined aswhere k is a concentration parameter and u is the mean direction and is a normalization constant. In the case of a diagonal matrix A, the Fisher–Bingham distribution is also known as Kent distribution [1,23].
We show the 2D and 3D versions of the peanut, ODF, Bingham, and von Mises–Fisher distributions in Figure 1.
1.4. Definitions of First and Second Moments
Since we will be calculating the first and second moments of the spherical distributions in n dimensions to obtain the expectation and the variance–covariance matrix, we provide the explicit definitions here. In general, the expectation [10] is defined as
and variance–covariance matrix [10] is defined as
Here, for denotes the tensor product between matrices. For simplicity of notation, we give names to the zeroth, first, and second moment. The zeroth moment is defined by
the first moment is defined by
and the second moment is defined by
2. First and Second Moments of von Mises–Fisher Distributions
In this section, we calculate the first and second moments of the general n-dimensional von Mises–Fisher distributions (5), in order to get general formulas for expectation and the variance–covariance matrix for these distributions.
For simplicity of notation, sums over crossed repeated indices are understood as in tensor calculus [10]
We also recommend referring to Appendix A.2, Appendix A.4 and Appendix A.5 for the basic properties of Bessel functions, definitions of and , as well as formulas that are used in the preceeding calculations.
Theorem 1.
Consider the von Mises–Fisher distribution (5) in any dimension n. The expectation and variance–covariance matrix are
Proof.
Expectation: We abbreviate the normalization constant in (5) as
Following a similar procedure as in [10] we calculate the expectation. Let be an arbitrary vector, then, using (5) we obtain
where we use the summation convention (15). Note, that is a unit vector and also the outside normal vector at on . Hence, we apply the divergence theorem on and continue the calculation as follows
where, in the third equivalence, we divide the integral on a ball into radial and angular components, and in the last step we applied (1).
Making use of the Bessel identities (A5) and (A6), we rewrite the term within the integral, that is
Using (21), we simplify further and apply the fundamental theorem of calculus to obtain
Therefore, we find that
After simplifying, and noting that b is an arbitrary vector, it follows that
Note that, from this calculation, we also obtain the following useful formula
by equating the right-hand term of the fourth equivalence in (20) with the right-hand term in the last equivalence of (22).
Second moment: We now calculate the second moment as well as the variance–covariance matrix for the von Mises–Fisher distribution (5).
Since the expectation for (5) is nonzero, we directly calculate the second term in the variance–covariance matrix formula (11). Using (23), it is simply
Now, we calculate the first term in the variance–covariance matrix formula (11), which is the second moment, by following the approach in [10].
Let c be defined by (18) and . Again, we use the fact that is the outside normal vector at on to apply the divergence theorem. Thus, we obtain
The first integral is solved in (24). We calculate the integral in the second term as
by applying (1) at the second equivalence.
By using the Bessel identities (A5) and (A6), we can rewrite the term in the integral as
Using (26) and (A5), we obtain
Thus,
Using (22) and (28), we find that
since are arbitrary.
□
Corollary 1.
Consider the bimodal von Mises–Fisher distribution
The expectation and the variance–covariance matrix for (31) is given by
Proof.
We can rewrite (31) as
where is defined by (5) and is also defined by (5), but with u replaced by . Using this, we can calculate the expectation and the variance–covariance matrix using the results in Theorem 1. The expectation is calculated as follows
Since the expectation is 0, the variance–covariance matrix is given by its second moment. Therefore, using (29), we obtain
□
Example for : The von Mises–Fisher distribution in two dimensions is called the von Mises distribution. It has been used in various applications that we mentioned above. Hence, here, we recall the result for the bimodal von Mises distribution in two dimensions [10]:
Example for : It is interesting to consider the important case of the von Mises distribution (5) for . For , we find
In [10], these terms were found as
Hence, we can compare the coefficients and find three new identities for Bessel functions:
Note that (37) is equivalent with (38) for . These formulas can also be derived by using the trigonometric form of Bessel function identities for , , defined in [24], where
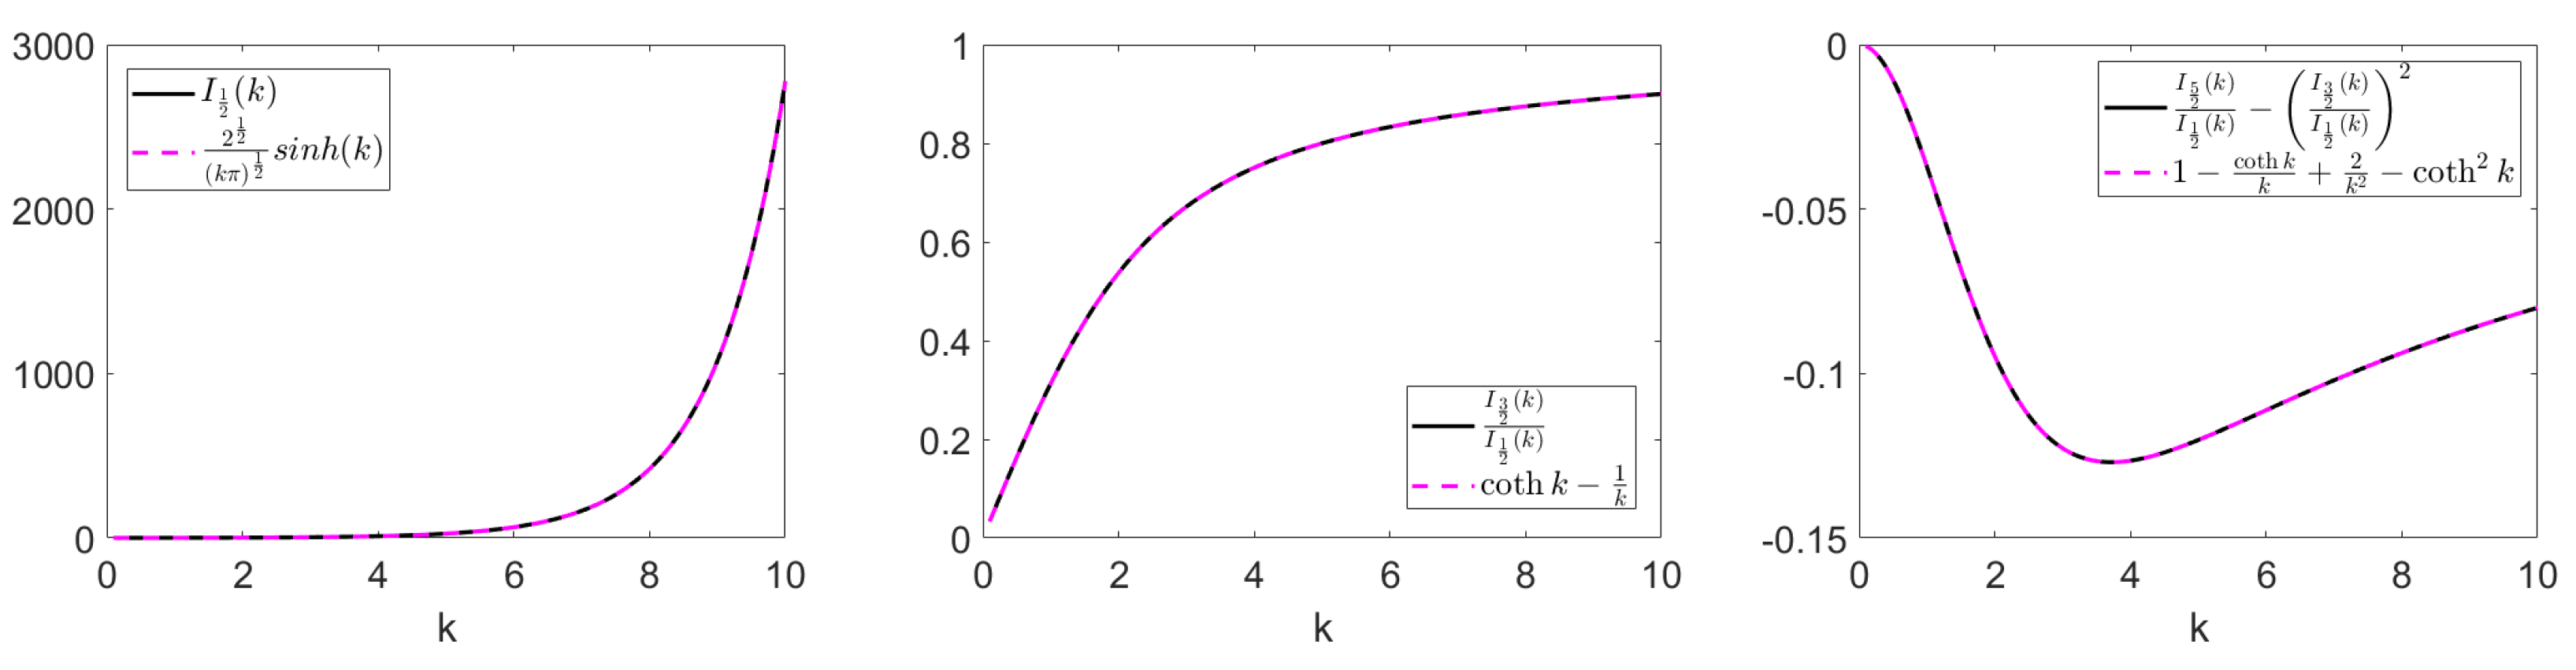
We confirm that the above identities hold numerically in Figure 2.
Figure 2.
The black curve in the left, middle, and left images illustrates the left−hand side of the Equations (40), (37), and (39). The dashed pink curve in the left, middle, and left images illustrates the right-hand side of the Equations (40), (37), and (39). The images show numerical agreement between both sides of the equivalences (40), (37), and (39).
Summary of Section 2
In this section, we computed the first and second moments of the von Mises–Fisher distribution (5) in the proof of Theorem 1 to obtain the explicit forms of the expectation and variance–covariance matrix for n dimensions. To our knowledge, these formulas for the expectation and the variance–covariance matrix in the general dimension n are new. Corollary 1 provides a method on how to generalize the explicit formulas in Theorem 1 to obtain the analytical form of the expectation and variance–covariance matrix for mixed modal von Mises–Fisher distributions, where we used the bimodal von Mises–Fisher distribution as an example. In this section, we also find new versions of Bessel function identities as a side result.
3. First and Second Moment of Peanut Distribution
We first note that the peanut distribution (6), the ODF (7), and the Bingham distribution (8) are all of the form
with an appropriate function F, where A is a given matrix. In the case of ODF, we actually use , but the structure is the same. Due to symmetry in , the first moment equals zero:
Lemma 1.
If A is a given matrix and q is of the form , then . Moreover, all odd moments are zero too.
Proof.
Let denote the first coordinate of in . We split the sphere according to the positive and negative component, obtaining two hemispheres:
This allows us to exploit symmetry to get the following result
□
- For the second moment, we consider each distribution separately.
3.1. Second Moment of the Peanut Distribution
Here, we calculate the variance–covariance matrix for the peanut distribution (6). Note that, since , the variance–covariance matrix is simply the second moment of (6), that is
With this, we can formulate our result, which to our knowledge is a new formula for the variance–covariance matrix of the peanut distribution (6) in n dimensions.
Theorem 2.
Proof.
We have seen in Lemma 1 that . For simplicity, we define the coefficient in (6) as
To compute the second moment, we multiply by two arbitrary vectors in order to obtain a scalar value. Then, we use the fact that is the outside normal vector at on to apply the divergence theorem. Using (6) and (44), we obtain the following result
where, in the third equivalence, the divergence theorem was applied and, in the last equivalence, the product rule was used.
Next, we simplify the final two terms in the above calculation. The first term simplifies as
since , implying that For the second term, we set
and simplify
In the above calculation, the divergence theorem was applied at the second equivalence and the last equivalence made use of (A10).
Therefore, since are arbitrary, it follows that
□
3.2. Summary of Section 3
In this section, we computed the first and second moments of the peanut distribution (6) to obtain explicit forms for the expectation and variance–covariance matrix in Theorem 6. To our knowledge, the analytical formulas for expectation and variance–covariance matrix for the peanut distribution are new. We also showed that spherical distributions in the form have . We applied the same method for the ODF and the Bingham distributions, but unfortunately, no closed-form expressions could be derived.
4. Eigenvalues and Anisotropy
When spherical distributions are used in diffusion models, the variance–covariance matrix describes the anisotropic movement of the random walkers [17]. The level of anisotropy can be measured by the eigenvalues of the diffusion tensor and by the fractional anisotropy () [7]. The fractional anisotropy is an index between 0 and 1, where 0 is the case of full radial symmetry giving isotropy and 1 is the case of extreme anisotropic alignment to a particular direction. Another indicator of anisotropy is the ratio R of the largest to the smallest eigenvalue of the diffusion tensor. This quantity ranges between 1 (isotropic) to ∞ (maximal anisotropic).
Note that the fractional anisotropy and the anisotropy ratio are only used for symmetric distributions of the form . In this case, and
Hence, the following applies to the peanut distribution and to the bimodal von Mises Fisher distribution (31). The ODF and the Bingham distributions are also symmetric, but since we do not have explicit forms of the second moments, we cannot compute their anisotropy values for general dimensions.
Recall that, in (4), we identified the diffusion tensor as
where s is the speed and is the turning rate of a cell or individual. Hence, the eigenvalues of are scaled versions of the eigenvalues of .
The fractional anisotropy (FA) formulas are defined separately for two and three dimensions and we summarize them in the following definition.
Definition 1.
- 1.
- The fractional anisotropy in two dimensions is given bywhere are the eigenvalues of a two-dimensional tensor and is the average of the two eigenvalues [7].
- 2.
- The fractional anisotropy in three dimensions is given bywhere are the eigenvalues of a three-dimensional tensor and is the average of the three eigenvalues [7].
- 3.
- The anisotropy ratio R is defined as
Theorem 3.
Proof.
The formulas for the fractional anisotropy follow directly, by substituting the eigenvalues of (51) into (48) and (49), respectively. The upper bound follows from taking . For the ratio R, we write
where the maximum eigenvalue and minimum eigenvalues of A are denoted by and , respectively. All other eigenvalues are called and the trace becomes the sum of the eigenvalues. □
It is very surprising to see that the anisotropy ratio is bounded by a finite value of 3 in any space dimension, and the fractional anisotropies are uniformly bounded by a value less than 1. This means the peanut distribution does not allow for arbitrary anisotropies, and for that reason it is of limited use in the modelling of biological movement data.
Next, we consider the anisotropy of the bimodal von Mises–Fisher distribution (31).
Theorem 4.
Proof.
To compute the eigenvalues for (55), we first take the vector u and show that it is indeed an eigenvector of (55), since
Hence, . Now, we take any (where ) and show that it is an eigenvector of (55) as well, since
Thus, is an eigenvector with an eigenvalue . Since we can define perpendicular vectors, we conclude that
The formulas for the anisotropies and for R follow from substituting the determined eigenvalues into the definitions. To determine the upper bounds for the formulas, we compute the limits of and . We start with the isotropic case of . We apply the expansion of Bessel functions as shown in (A4)
and
To evaluate the limit as , we apply the expansion (A7) for large k to obtain
and
Now, we compute the bounds for the ratio . We see that if , by the above calculations. Further, as , since
And finally,
So, and as . Further, and as . □
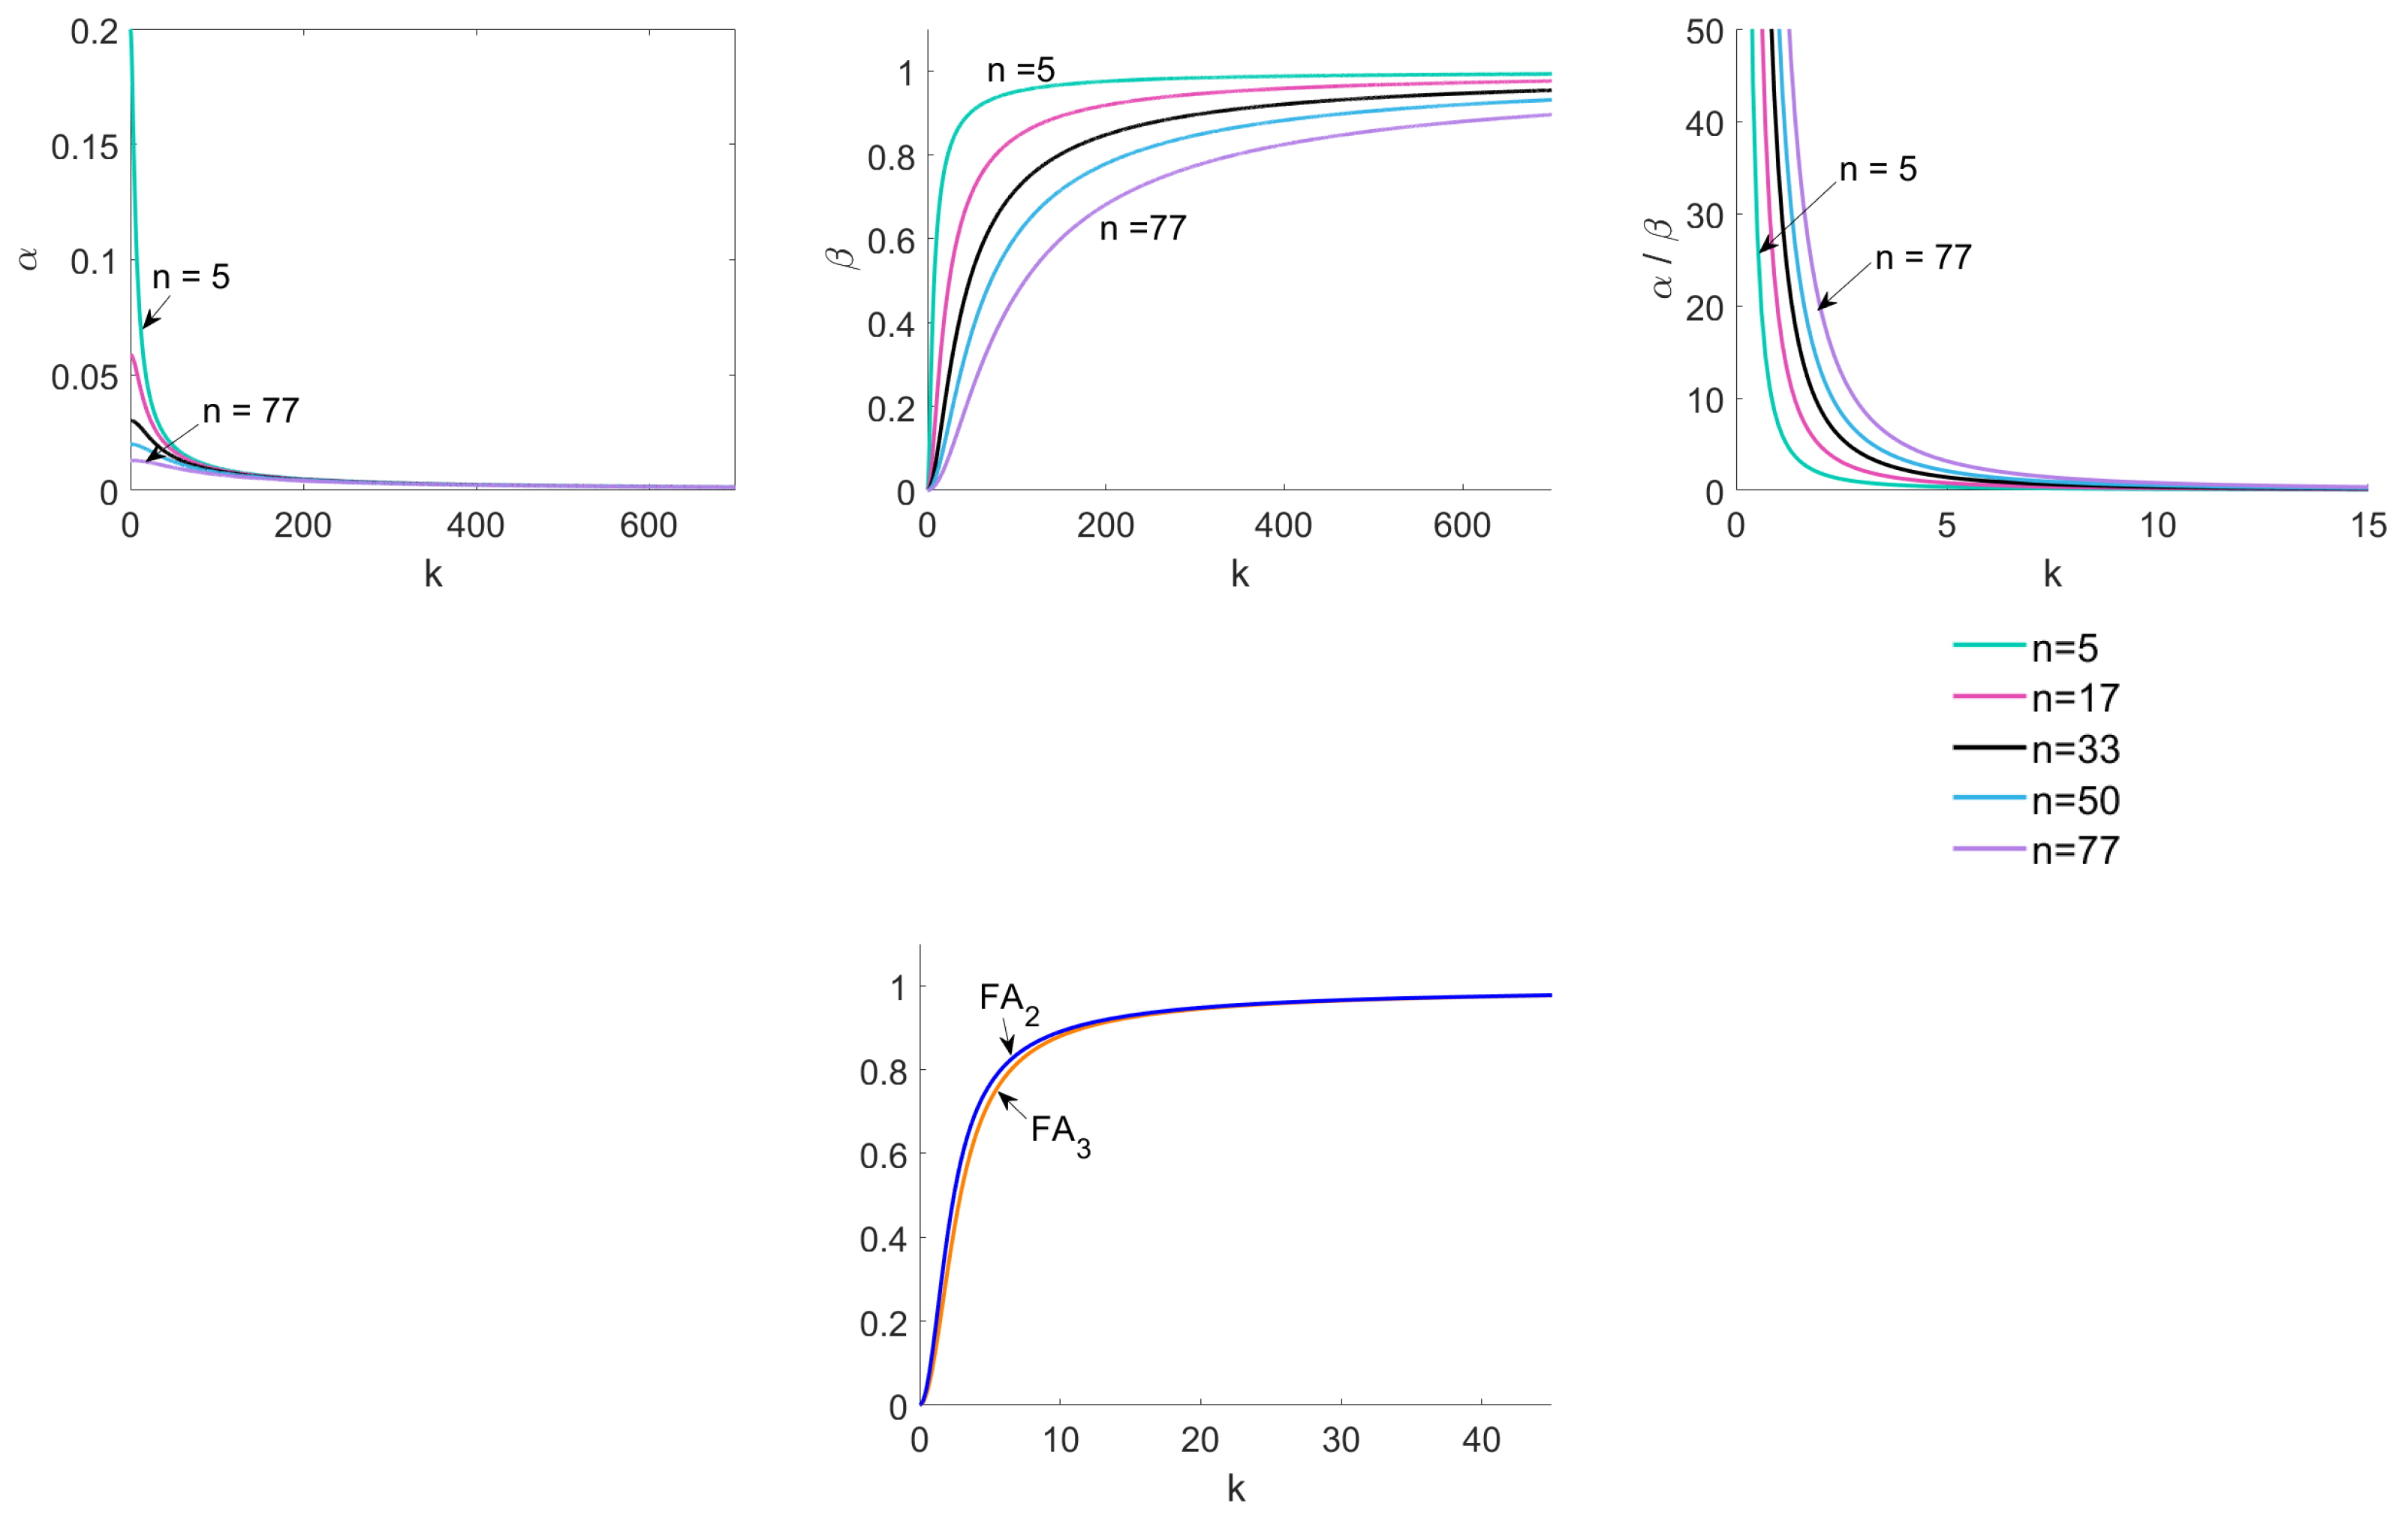
In Figure 3, we confirm our calculations numerically. We plot , , , , with respect to k and illustrate that they converge to the limits computed above. Note that, for some images in Figure 3, we truncated the intervals to see the functions more clearly.
Figure 3.
The top row illustrates , , and as for (see Theorem 4 for explicit forms of and ). The bottom image illustrates and as for dimensions and , respectively. In the bottom figure, the blue curve is and the orange curve is (see Theorem 4 for the definitions of and ). All images relate to the bimodal von Mises–Fisher distribution.
Summary
In this section, we computed the eigenvalues for the peanut (6) and the bimodal von Mises–Fisher distributions (31) for their respective diffusion tensors in Theorems 3 and 4. We also found explicit versions of the and formulas as well as the R ratio in Theorems 3 and 4. The , , and R formulas for the peanut distribution have been shown to be bounded, unlike for the von Mises–Fisher distribution.
5. An Illustrative Example of Glioma Spread
To illustrate the main results, we consider a glioma spread model in a simplified scenario. Glioma are highly aggressive brain tumors which invade into healthy tissue guided by white matter fibre tracks [25]. This process has been successfully modelled using Fisher–KPP-type equations (see model (66) below) [7,26,27]. The underlying anisotropy of white matter tracks can be measured through diffusion tensor MRI (DTI) [18,28,29], and this is where we start our illustrative example. We consider a two-dimensional domain and assume that a diffusion tensor is measured as
This indicates a strong bias in the x direction and much less movement in the y direction. The measurements of DTI record the movement of water molecules [18,29], which we need to transfer into a movement model for cancer cells. We do this using the transport equation approach mention in Section 1.1 and the peanut distribution and the bimodal von Mises distributions, respectively. Both methods will give us an effective diffusion tensor for the glioma cells.
We also assume, for simplification, that movement speed and turning rate are normalized such that .
Taking A from above, with , we compute the two-dimensional diffusion tensor of the peanut distribution (51) as
To compute the corresponding diffusion tensor for the bimodal von Mises distribution (55) for , we need the dominant eigenvector u and the concentration parameter k. In [7], the model was fit to glioma patient data and it was found that the concentration parameter k is about 3–5 times the fractional anisotropy of the patients DTI data. Hence, here, we assume
The dominant direction is . Then, from (36) we find
We see immediately that the von Mises tensor is more anisotropic than the peanut tensor above.
We now take these two diffusion tensors, (64) and (65), and an isotropic tensor, , for comparison and solve the corresponding anisotropic glioma model [7]
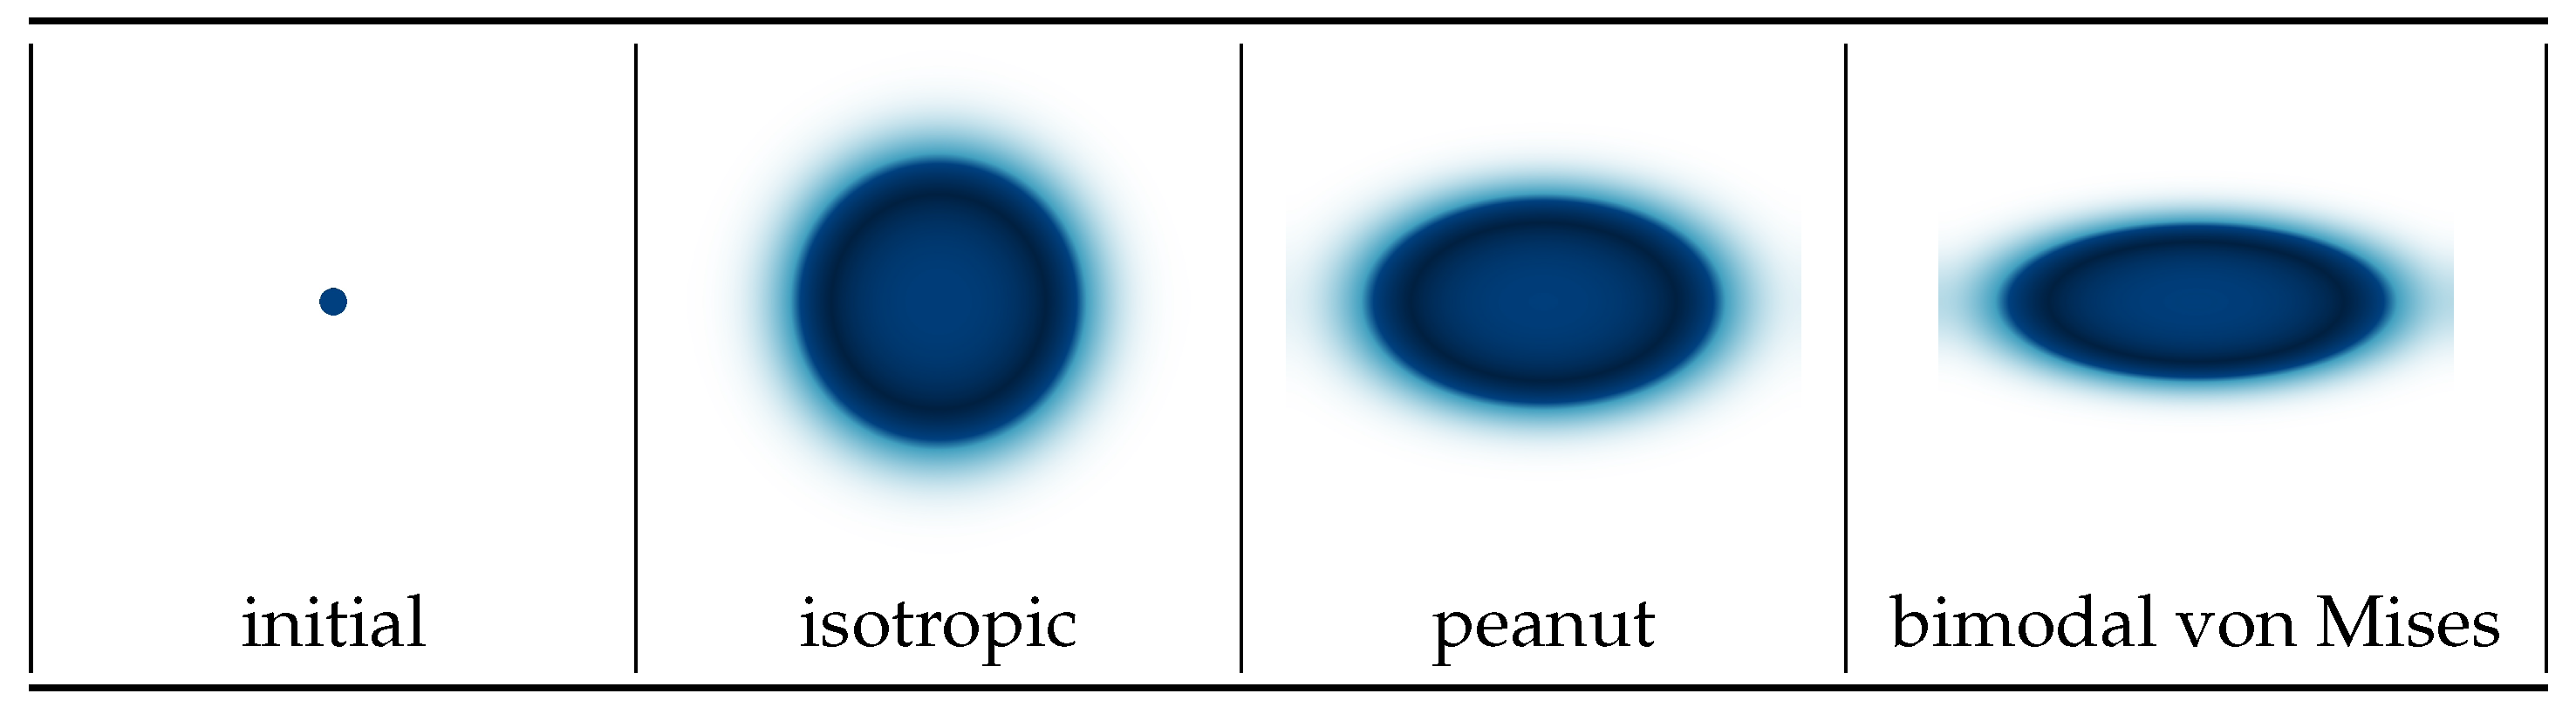
on a square domain with no-flux boundary conditions. Here describes the glioma cell density as a function of space and time and r is the maximal cancer growth rate. We choose and we initialize the simulation with a small cancer seed in the middle of the domain. In Figure 4, we show the initial condition and the model results after 40 time units. We see that the von Mises distribution is able to describe a stronger directional bias as compared to the peanut. Note that, for this example, A does not change with space and remains constant at any given spatial point, meaning that this example is applicable to a small region in the tissue, such as a small section of a white matter tract in the brain. For larger domains, like the entire brain, depends on space, and a more detailed modelling is needed. This was done, for example, in [7,11,20].
Figure 4.
Initial condition and simulations of glioma spread of model (66) at time on a square domain, using three different diffusion tensors, the isotropic tensor, the peanut, and the bimodal von Mises. Here, blue indicates maximum tumor density, while white indicates healthy tissue.
6. Discussion
The standard way to compute moments of spherical distributions would be to use polar coordinates and engage in a series of trigonometric integrations. While this is often possible in two and three dimensions, it gets tedious, or impossible, in higher dimensions. Here, we present an alternative method that can be used in any space dimension. This method was first used in [10] in two and three dimensions. It uses the divergence theorem on the unit ball to transform and simplify the integrals as much as possible. As a result, we obtain explicit formulas for the variance–covariance matrices of the n-dimensional von Mises–Fisher distribution (Theorem 1) and the n-dimensional peanut distribution (Theorem 2) as new results. The formulas derived in Theorems 1 and 2 involve Bessel functions, which are standard functions in any software package. Hence, the numerical implementation of these formulas is straightforward. We tried to apply the method for computing the first and second moments of other spherical distributions such as the ordinary distribution function (ODF) (7) and the Bingham distribution (8), which, unfortunately, did not lead to closed form expressions. However, because Bingham and ODF distributions are symmetric, we do show that their expectation is zero. We also note that, based on our experience, Bingham and Kent distributions have not been used in the biological context yet. They seem to be more relevant in geophysical applications [30]. Hence, they are not the main focus of our paper.
Once the variance–covariance matrices were established, we considered levels of anisotropy as measured through the fractional anisotropies and the ratio of maximal over minimal eigenvalues. Surprisingly, the anisotropy of the peanut distribution is bounded away from 1 (Theorem 3) making it problematic to use in modelling. The anisotropy of the von Mises–Fisher distribution covers the entire range from isotropic to fully anisotropic (Theorem 4), and seems to have no restriction if used for modelling.
Using the explicit formulas derived here will significantly decrease the computation time in problems having a large amount of data that require a higher-dimensional von Mises–Fisher distribution [31] and decrease the computation time when simulating the transport equations (partial differential equations) that utilize the biological movement data [3,4,7]. Moreover, the formulas derived for the generalized von Mises–Fisher distribution can be easily extended to compute the expectation and variance covariance matrices of mixed von Mises–Fisher distributions by substituting the appropriate directional vectors and adding up the terms.
As we compute the higher dimensional integrals, we showcase a geometric interpretation of these integrals and the use of the divergence theorem. Hence, we combine the theory of distributions with calculus in a new way. Besides our explicit formulas, we believe our approach can open the door for further computations of explicit formulas for expectation, variance, and even higher moments of spherical distributions and enable further applications in biology.
Author Contributions
Conceptualization, A.S. and T.H.; Proof development, A.S.; Figure 1, Figure 2 and Figure 3, A.S.; Figure 4, T.H.; Writing—original draft preparation, A.S. and T.H.; Writing—review and editing, A.S. and T.H.; Supervision, T.H. All authors have read and agreed to the published version of the manuscript.
Funding
This research was funded by Natural Science and Engineering Research Council of Canada (NSERC) grant number RGPIN-2023-04269.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding author.
Acknowledgments
AS acknowledges the funding from the Alberta Graduate Excellence Scholarship and The Maud Menten Institute Accelerator award (PRN2). TH is supported through a discovery grant of the Natural Science and Engineering Research Council of Canada (NSERC), RGPIN-2023-04269.
Conflicts of Interest
The authors declare no conflicts of interest.
Appendix A
Appendix A.1. Derivation of the von Mises–Fisher Distribution
In [1], the von Mises–Fisher distribution is defined as the probability density
with respect to the uniform distribution on . The parameters in have the same interpretation as in (5). If we use the standard Lebesgue measure on , we divide (A1) by , and obtain the probability density (5). We can see this by the following calculation
where we made use of (A8) and (A9).
Appendix A.2. Modified Bessel Functions of First Kind
The von Mises–Fisher distribution (5) has a modified Bessel function of first kind appearing in the normalization factor. Here, we state the definitions of the Bessel function of first kind and the modified Bessel function of first kind of order p () as well as list some useful identities.
The Bessel function and modified Bessel function of first kind can be defined as follows [32]
where , .
Bessel functions have many identities [24]. We will use the following ones often in our calculations
where . See Appendix A.3 for the proofs of these identities.
We will also make use of the following expansion for large , [33]
for fractional and integer orders p.
Appendix A.3. Bessel Function Identities Proofs
Identity (A5) follows through the following calculation
since .
Appendix A.4. n-Ball and (n − 1)-Sphere
The surface area of an n-sphere, , and the volume of an n-ball, , appear often in our calculations. Here, we recall these formulas explicitly [34]
where is the gamma function. See [34] for more details as to how the formulas in (A8) were derived.
The gamma function has the following identity [35], which we will use often
Using (A9) it is easy to see that
Appendix A.5. Matrix Derivative
We denote by an operator that performs the gradient with respect to , that is, . It follows that
where The identity (A11) can be computed as follows. Since
and
it follows that
References
- Mardia, K.V.; Jupp, P.E. Directional Statistics; John Wiley & Sons: Hoboken, NJ, USA, 2009. [Google Scholar]
- McKenzie, H.W.; Merrill, E.H.; Spiteri, R.J.; Lewis, M.A. How linear features alter predator movement and the functional response. Interface Focus 2012, 2, 205–216. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Painter, K.J.; Hillen, T. Navigating the flow: Individual and continuum models for homing in flowing environments. J. R. Soc. Interface 2015, 12, 20150647. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Painter, K.J. Multiscale models for movement in oriented environments and their application to hilltopping in butterflies. Theor. Ecol. 2014, 7, 53–75. [Google Scholar] [CrossRef] [Scilit]
- Johnston, S.T.; Painter, K.J. Avoidance, confusion or solitude? Modelling how noise pollution affects whale migration. Mov. Ecol. 2024, 12, 17. [Google Scholar] [CrossRef] [Scilit]
- Friedl, P.; Bröcker, E.B. The biology of cell locomotion within three-dimensional extracellular matrix. Cell. Mol. Life Sci. CMLS 2000, 57, 41–64. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Swan, A.; Hillen, T.; Bowman, J.C.; Murtha, A.D. A patient-specific anisotropic diffusion model for brain tumour spread. Bull. Math. Biol. 2018, 80, 1259–1291. [Google Scholar] [CrossRef] [Scilit]
- Painter, K.J.; Hillen, T. From random walks to fully anisotropic diffusion models for cell and animal movement. In Cell Movement: Modeling and Applications; Springer: Berlin/Heidelberg, Germany, 2018; pp. 103–141. [Google Scholar] [CrossRef] [Scilit]
- Wolf, K.; Müller, R.; Borgmann, S.; Brocker, E.B.; Friedl, P. Amoeboid shape change and contact guidance: T-lymphocyte crawling through fibrillar collagen is independent of matrix remodeling by MMPs and other proteases. Blood 2003, 102, 3262–3269. [Google Scholar] [CrossRef] [Scilit]
- Hillen, T.; Painter, K.J.; Swan, A.C.; Murtha, A.D. Moments of von Mises and Fisher distributions and applications. Math. Biosci. Eng. 2017, 14, 673–694. [Google Scholar] [CrossRef] [Scilit]
- Painter, K.; Hillen, T. Mathematical modelling of glioma growth: The use of diffusion tensor imaging (DTI) data to predict the anisotropic pathways of cancer invasion. J. Theor. Biol. 2013, 323, 25–39. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Conte, M.; Surulescu, C. Mathematical modeling of glioma invasion: Acid-and vasculature mediated go-or-grow dichotomy and the influence of tissue anisotropy. Appl. Math. Comput. 2021, 407, 126305. [Google Scholar] [CrossRef] [Scilit]
- Finnegan, L.; Pigeon, K.E.; Cranston, J.; Hebblewhite, M.; Musiani, M.; Neufeld, L.; Schmiegelow, F.; Duval, J.; Stenhouse, G.B. Natural regeneration on seismic lines influences movement behaviour of wolves and grizzly bears. PLoS ONE 2018, 13, e0195480. [Google Scholar] [CrossRef] [Scilit]
- McKenzie, H.W.; Lewis, M.A.; Merrill, E.H. First passage time analysis of animal movement and insights into the functional response. Bull. Math. Biol. 2009, 71, 107–129. [Google Scholar] [CrossRef] [Scilit]
- Othmer, H.G.; Dunbar, S.R.; Alt, W. Models of dispersal in biological systems. J. Math. Biol. 1988, 26, 263–298. [Google Scholar] [CrossRef] [Scilit]
- Othmer, H.G.; Hillen, T. The diffusion limit of transport equations derived from velocity-jump processes. SIAM J. Appl. Math. 2000, 61, 751–775. [Google Scholar] [CrossRef] [Scilit]
- Hillen, T. M5 mesoscopic and macroscopic models for mesenchymal motion. J. Math. Biol. 2006, 53, 585–616. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- O’Donnell, L.J.; Westin, C.F. An introduction to diffusion tensor image analysis. Neurosurg. Clin. 2011, 22, 185–196. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Douaud, G.; Jbabdi, S.; Behrens, T.E.; Menke, R.A.; Gass, A.; Monsch, A.U.; Rao, A.; Whitcher, B.; Kindlmann, G.; Matthews, P.M.; et al. DTI measures in crossing-fibre areas: Increased diffusion anisotropy reveals early white matter alteration in MCI and mild Alzheimer’s disease. Neuroimage 2011, 55, 880–890. [Google Scholar] [CrossRef] [Scilit]
- Engwer, C.; Hunt, A. Surulescu, C. Effective equations for anisotropic glioma spread with proliferation: A multiscale approach and comparisons with previous settings. Math. Med. Biol. 2016, 33, 435–459. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aganj, I.; Lenglet, C.; Sapiro, G.; Yacoub, E.; Ugurbil, K.; Harel, N. Reconstruction of the orientation distribution function in single-and multiple-shell q-ball imaging within constant solid angle. Magn. Reson. Med. 2010, 64, 554–566. [Google Scholar] [CrossRef] [Scilit]
- Basser, P.J. Diffusion and diffusion tensor MR imaging: Fundamentals. In Magnetic Resonance Imaging of the Brain and Spine; Lippincott Williams and Wilkins: Philadelphia, PA, USA, 2008; pp. 1752–1767. [Google Scholar]
- Kent, J.T. The Fisher-Bingham distribution on the sphere. J. R. Stat. Soc. Ser. B (Methodol.) 1982, 44, 71–80. [Google Scholar] [CrossRef] [Scilit]
- Abramowitz, M.; Stegun, I.A. Handbook of Mathematical Functions with Formulas, Graphs, and Mathematical Tables; US Government Printing Office: Washington, DC, USA, 1968; Volume 55.
- Giese, A.; Kluwe, L.; Laube, B.; Meissner, H.; Berens, M.E.; Westphal, M. Migration of human glioma cells on myelin. Neurosurgery 1996, 38, 755–764. [Google Scholar] [CrossRef] [Scilit]
- Swanson, K.R.; Alvord, E.C., Jr.; Murray, J.D. A Quantitative Model for Differential Motility of Gliomas in Grey and White Matter. Cell Prolif. 2000, 33, 317–329. [Google Scholar] [CrossRef] [Scilit]
- Konukoglu, E.; Clatz, O.; Bondiau, P.; Delignette, H.; Ayache, N. Extrapolation glioma invasion margin in brain magnetic resonance images: Suggesting new irradiation margins. Med. Image Anal. 2010, 14, 111–125. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Berenschot, G. Visualization of Diffusion Tensor Imaging. Master’s Thesis, Eindhoven University of Technology, Eindhoven, The Netherlands, 2003. [Google Scholar]
- Beaulieu, C. The basis of anisotropic water diffusion in the nervous system—A technical review. NMR Biomed. 2002, 15, 435–455. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fallaize, C.J.; Kypraios, T. Bayesian Model Choice for Directional Data. J. Comput. Graph. Stat. 2024, 33, 25–34. [Google Scholar] [CrossRef] [Scilit]
- Banerjee, A.; Dhillon, I.S.; Ghosh, J.; Sra, S.; Ridgeway, G. Clustering on the Unit Hypersphere using von Mises-Fisher Distributions. J. Mach. Learn. Res. 2005, 6, 1345–1382. [Google Scholar]
- Baricz, Á. Generalized Bessel Functions of the First Kind; Springer: Berlin/Heidelberg, Germany, 2010. [Google Scholar]
- Olver, F.W. NIST Handbook of Mathematical Functions Hardback and CD-ROM; Cambridge University Press: Cambridge, MA, USA, 2010. [Google Scholar]
- Folland, G.B. How to integrate a polynomial over a sphere. Am. Math. Mon. 2001, 108, 446–448. [Google Scholar] [CrossRef]
- Sebah, P.; Gourdon, X. Introduction to the gamma function. Am. J. Sci. Res. 2002, 2–18. [Google Scholar]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).