


Abstract
Thousands of unique noncoding RNAs (ncRNAs) exist within the genomes of higher eukaryotes. Upon virus infection, the host generates interferons (IFNs), which initiate the expression of hundreds of interferon-stimulated genes (ISGs) through IFN receptors on the cell surface, establishing a barrier as the host’s antiviral innate immunity. With the development of novel RNA-sequencing technology, many IFN-induced ncRNAs have been identified, and increasing attention has been given to their functions as regulators involved in the antiviral innate immune response. IFN-induced ncRNAs regulate the expression of viral proteins, IFNs, and ISGs, as well as host genes that are critical for viral replication, cytokine and chemokine production, and signaling pathway activation. This review summarizes the complex regulatory role of IFN-induced ncRNAs in antiviral innate immunity from the above aspects, aiming to improve understanding of ncRNAs and provide reference for the basic research of antiviral innate immunity.
Following Crick’s central dogma [1,2], genetic information is passed from DNA to RNA, which is then translated into proteins. Over many years, proteins have been widely recognized as the final products that perform the main functions encoded by genes, though protein-coding genes occupy <2% of the human genome. As sequencing technology advances, other products of the human genome are coming into view, revealing the “dark energy” of DNA. According to the NIH ENCODE project results, approximately 80% of the human genome is endowed with biochemical functions and, interestingly, about 62% of genes are transcribed into noncoding RNAs (ncRNAs) [3]. Upon viral infection or interferon (IFN) stimulation, many ncRNAs are generated to regulate various vital cellular processes, including pre-transcriptional, transcriptional, and post-transcriptional regulatory processes. Numerous ncRNAs are reported to be involved in antiviral activities, most of which are microRNAs (miRNAs), long ncRNAs (lncRNAs), or circular RNAs (circRNAs).
IFN was originally discovered as an infection-inhibiting factor. Subsequently, IFN-specific inducible mRNAs and proteins were identified. The canonical interpretation of IFN-mediated antiviral innate immune responses suggests that IFNs induce the transcription of IFN-stimulated genes (ISGs), which further alter the proteome in cells and establish an antiviral cellular state [4]. However, according to recent studies, IFN-mediated antiviral innate immune responses may be a more complex process than transcriptional induction of ISGs. Initially, researchers mainly detected IFN-induced gene expression by surveying IFN-stimulated transcriptome changes through microarray technology, which enabled the detection of the enrichment of select mRNAs through poly(A) affinity or arrays used to probe for transcripts of encoded proteins [5,6,7]. Thus, they were unable to capture ncRNAs that were not polyadenylated, such as miRNAs, circRNAs, piwi-interacting RNAs (piRNAs), and enhancer RNAs (eRNAs, which are lncRNAs) [7,8,9,10]. Polyadenylated lncRNAs have been frequently dismissed as “garbage” because they do not encode proteins. However, an increasing number of studies indicate that IFNs can induce some ncRNAs to participate in antiviral innate immunity [11,12,13,14,15]. These results demonstrate the biogenesis of ncRNAs and the role of ncRNAs, enhancing our understanding of these molecules and serving as fundamental concepts to guide antiviral innate immunity.
3. Discussion
3.1. Validation of IFN-Induced NcRNAs Complements the Traditional Definition of ISGs
IFNs trigger the transcription of ISGs, change the protein composition of host cells, and mediate the antiviral state. Although IFN-mediated antiviral innate immunity has been studied for many years, more research is needed to understand IFN-regulated antiviral mechanisms. Many recent discoveries in infectomics based on contemporary sequencing and proteomic techniques have changed our understanding of IFN-related biology [4,30,76]. In a narrow sense, ISG expression is up-regulated at the transcriptional level in response to stimulation with IFN, a direct target of the IFN signaling pathway. ISGs have traditionally been thought to function through the proteins they encode, but recent studies have shown that they can also exert antiviral functions through the ncRNAs they transcribe [13,29,30,42,43]. Peng et al. [77] detected that widespread differentially expressed (DE) lncRNAs respond to virus infection and regulate the host’s innate immune response by sequencing analysis. Interestingly, most up-regulated DE lncRNAs after viral infection are also significantly up-regulated by IFN-α treatment [30,77]. Therefore, promoter analysis and expression correlation studies suggest that these lncRNAs might be ISGs [30]. For example, a recent study used ChIPBase v2.0 to reveal that the expression of lncRNAs in SARS-CoV-2-infected cells might regulate STAT1, STAT3, and IFN regulatory factors [78]. These studies have updated our understanding of the biological landscape of IFNs and lncRNAs.
Andrew et al. investigated the presence of IFN-induced ncRNAs in human cells. They found hundreds of DE ncRNAs, but by analyzing ISG-encoded transcript types, a total of 90% and 92% of up-and down-regulated genes were classified as protein-coding genes, respectively [79]. Along these lines, we propose that IFN-induced ncRNAs complement ISG products. As genome annotation becomes more complete and more ncRNAs are discovered, a deeper understanding of the role of ncRNAs in antiviral innate immunity will become possible. Of note, the expression of many ISGs is induced by IFNs, viral infection, double-stranded RNA, and signaling pathways [80]. Therefore, studying IFN-induced ISGs and ISGs triggered by pathogenic microorganisms will help to discover ISGs and reveal their antiviral mechanisms.
3.2. Diversity of IFN-Induced NcRNAs
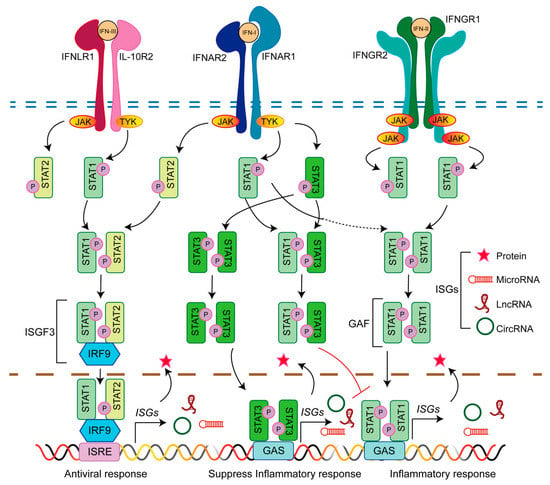
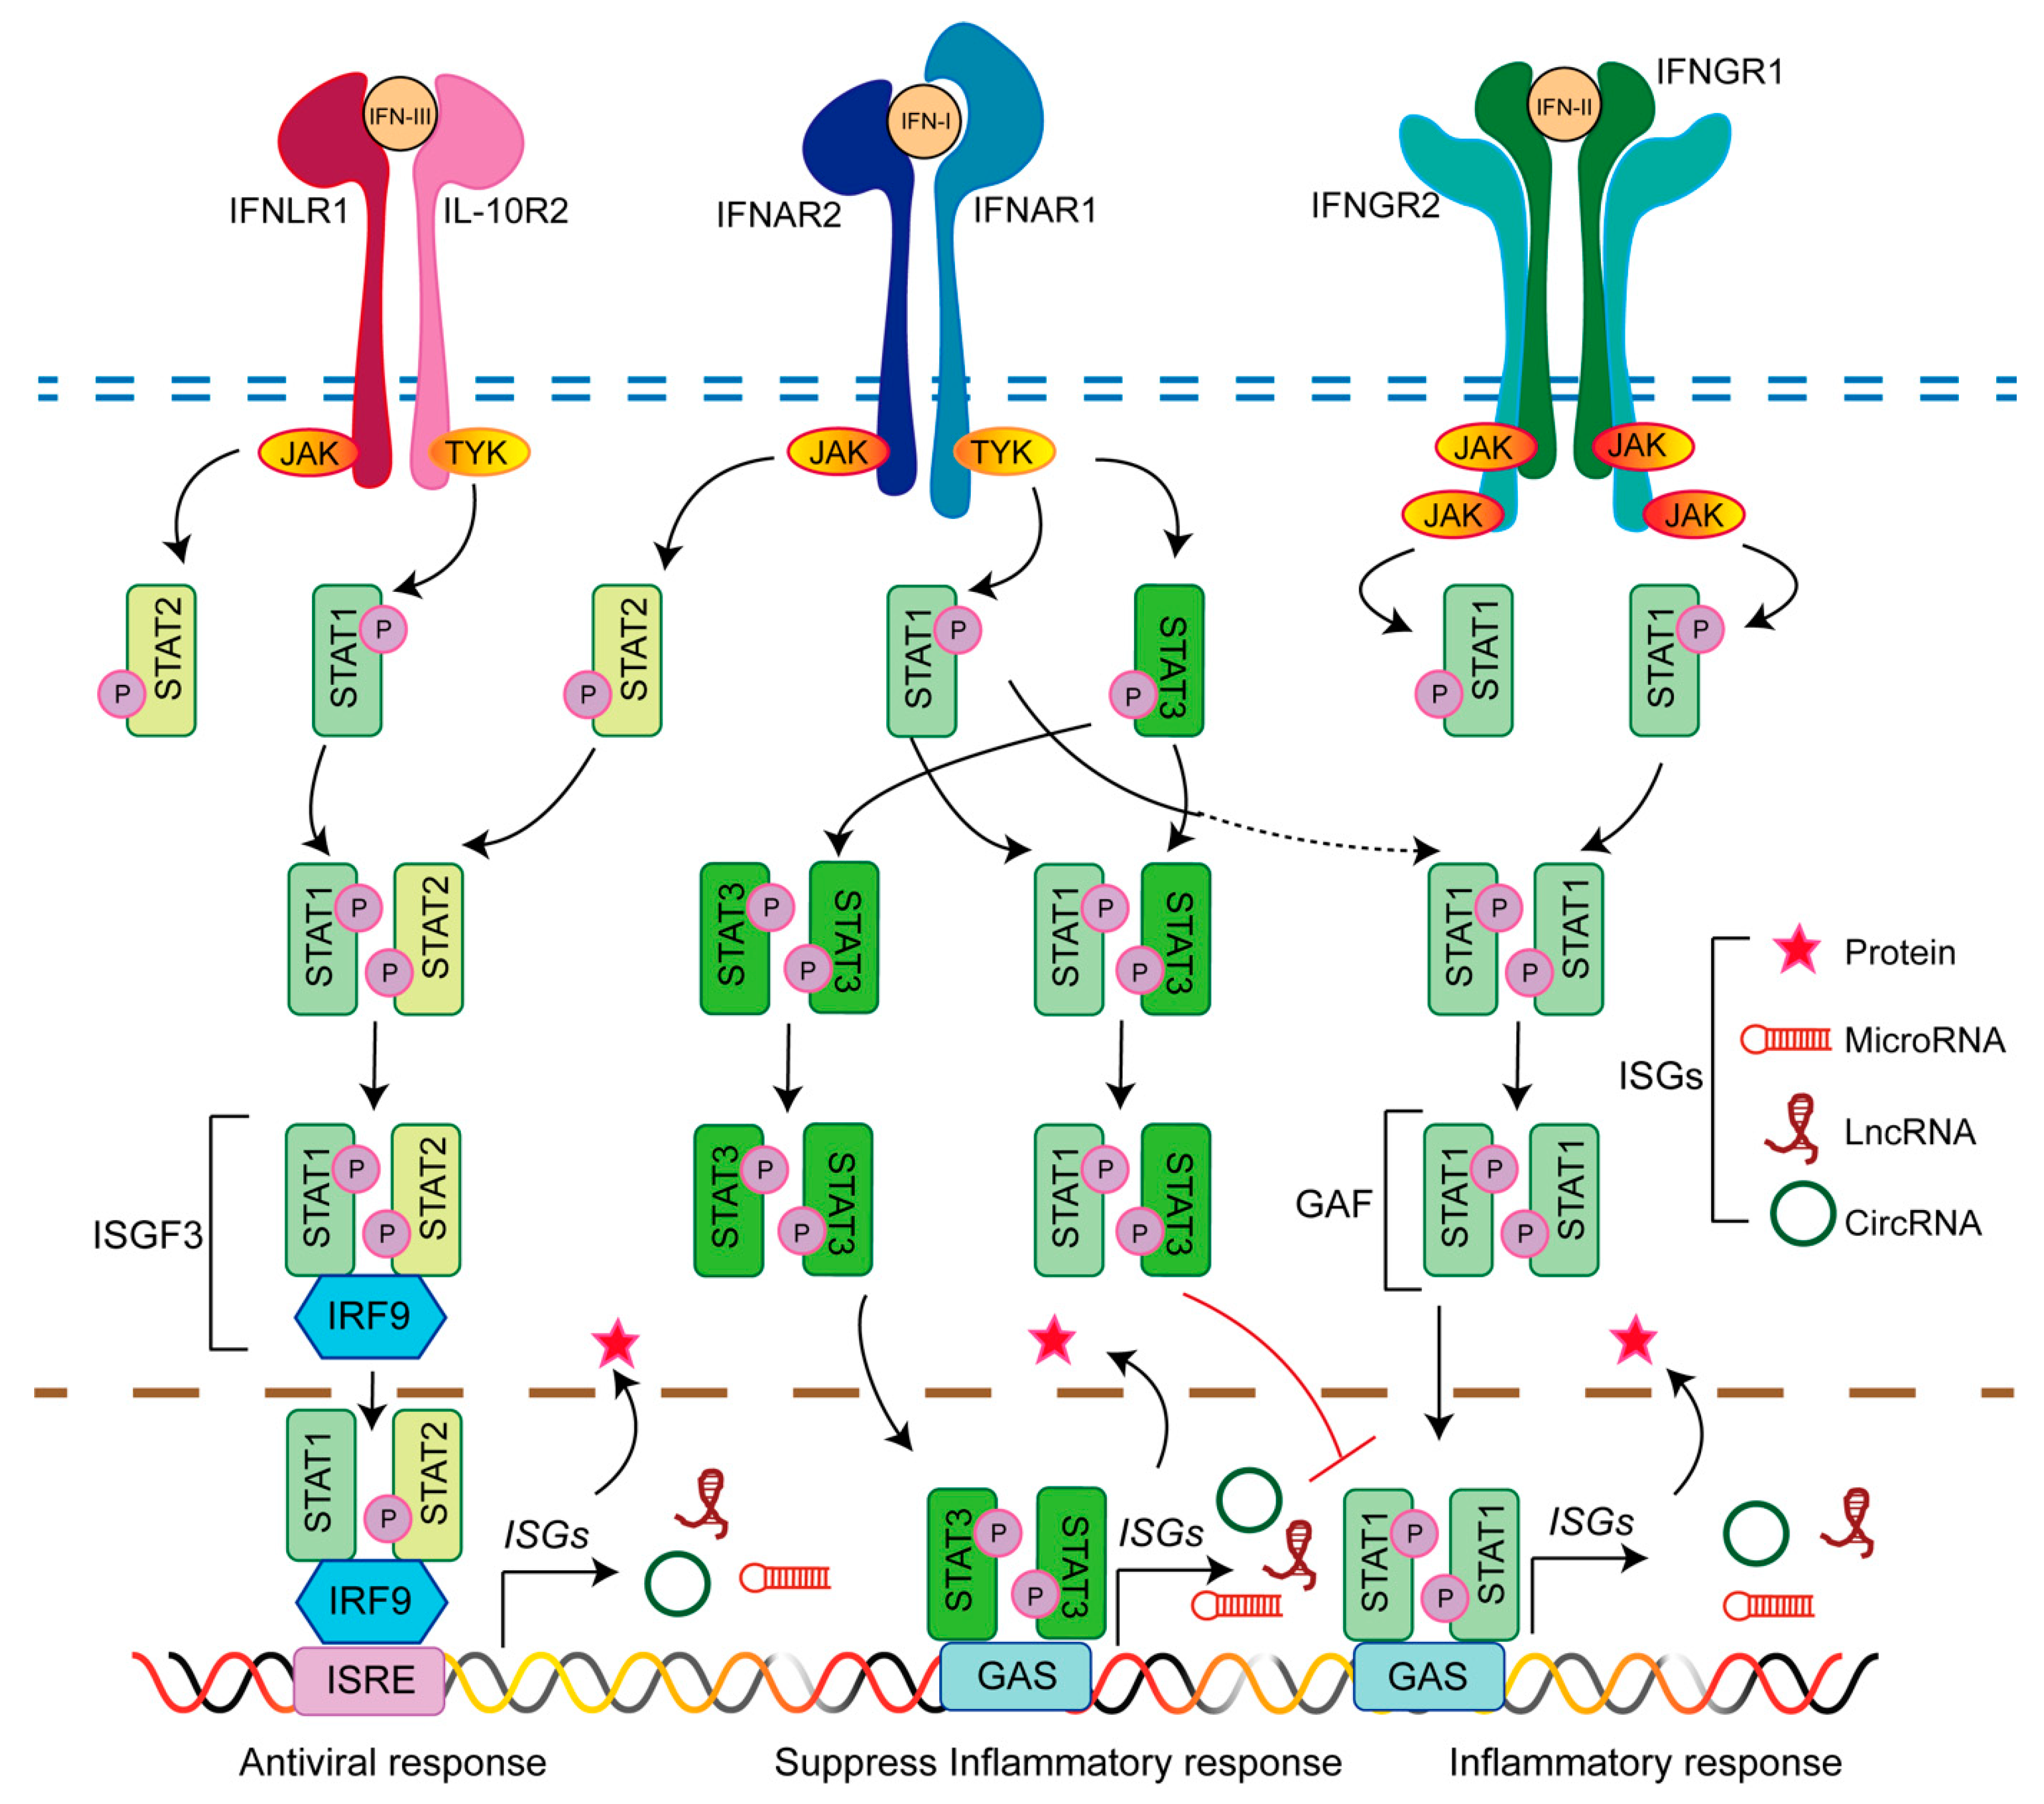
The dozens of IFNs are classified into three categories. The classification of IFNs may lead to the diversity of IFN-induced ncRNAs. As seen in Figure 1, IFNs activate multiple signaling pathways through different receptors. Different signaling pathways stimulated by IFNs may induce different ncRNAs. Although the type I and type III IFN genes are distinct and bind to different receptors, they are induced by the same pathologic route of infection and activate the expression of relevant antiviral, antiproliferative, and immunoregulatory genes. Although IFN-γ is derived only from immune cells, its receptor is expressed at moderate or low levels in almost all cell types [23]. The structure of type II IFNs is independent of that of type I and III IFNs, but it induces the same transcription of some ISGs as that induced by type I IFNs [81]. Moreover, type I IFN signaling initiates IFN-γ signaling [82]. In addition, the distribution of receptors in different cells may be the reason ncRNAs exhibit specific expression patterns that depend on cell or tissue type. These results suggest that IFN-induced ncRNAs are diverse, but some of them can be induced by all types of IFNs, which may play a more important role in antiviral immunity responses.
The expression of ncRNAs largely depends on the cell type and is tightly controlled by various cellular signaling pathways. Because different IFNs induce the expression of different proteins, different IFNs specifically induce the expression of various ncRNAs. For example, numerous ISG-encoded proteins inhibit HCV replication. However, certain ISG-encoded proteins, such as ISG15 and USP18, promote HCV replication. Thus, ncRNAs act as positive or negative regulators to orchestrate a complex network and balance the IFN response, similar to the effect of ISG-encoded proteins. Furthermore, high-throughput sequencing of the transcriptome reveals that sequences in ncRNAs are similar to those reported to be in ISGs, suggesting that they originate from the transcription of the same genes. The ncRNA network of ISGs may help extend our understanding of the innate immune system against viruses. Whether IFN-stimulated ncRNAs interact with IFN-stimulated proteins to play a synergistic or antagonistic role in innate immunity remains to be further investigated.
3.3. Specificity of NcRNAs Induced by a Viral Infection
The characterization of ncRNAs not only provides a novel model for host defense in mammalian cells, but has also enabled the identification of novel components that can be added to the repertoire of antiviral effectors. Similar to the lncRNA VIN [83], these ncRNAs are induced only by specific viruses and are not affected by a general viral or IFN response, which is associated with differences in virulence. Additionally, some ncRNAs are not expressed at the same level when stimulated by different viruses, and some play opposite roles in the antiviral response. For example, lncRNA NEAT1 is up-regulated by HIV-1 [84,85], Herpes simplex virus (HSV) [86,87], HTNV [88], hepatitis D virus [89], and IAV [86], but down-regulated by severe dengue virus [90]. In general, up-regulation of lncRNA NEAT1 expression appears to be a general response to viral infection. However, by promoting HSV infectivity, lncRNA NEAT1 inhibits the replication of other viruses. Whether the consequences promote or inhibit viral infection depends on downstream mechanisms.
3.4. Others Potential Effects of NcRNAs on Host Antiviral Innate Immunity
Many recent advances have been made in identifying ncRNA modifications and have been used to study their effects on lncRNAs and circRNAs, in addition to ribosomal RNAs (rRNAs) and tRNAs [91]. The methylation of adenosine at the N6 position in mammalian RNA is a highly abundant RNA base modification that promotes efficient initiation of translation of circular RNA proteins, participates in cellular activities, or performs other functions [92]. Therefore, we wondered whether different RNA modifications of IFN-stimulated ncRNAs could affect ncRNA function in antiviral immunity. IFN-stimulated ncRNAs are translated whether or not they participate in antiviral immunity through peptides. However, whether IFN-stimulated ncRNAs directly exert antiviral effects by targeting viral proteins remain to be determined. Both circRNAs and lncRNAs interact with miRNAs to perform various biological functions. Numerous circRNA–miRNA–mRNA interactions have been identified in viral infection, but the functions of these interaction networks remain to be further explored. Furthermore, whether IFNs induce certain other ncRNAs, such as snRNAs, rRNAs, piRNAs, and/or tRNAs, to participate in antiviral innate immunity is a worthy direction for future research. Indeed, determining whether IFNs induce these RNAs to participate in antiviral innate immunity and whether they form interaction networks warrants further investigation.
4. Conclusions
Given the role of IFN-stimulated ncRNAs in antiviral immunity, which enriches our understanding of IFN-mediated antiviral innate immunity, we were interested in determining the function of IFN-induced antiviral ncRNAs as ISGs. The IFN-stimulated miRNAs can directly target viral transcript or indirectly affect host protein expression to take part in antiviral innate immunity. The IFN-stimulated lncRNAs regulate gene expression on translation in cis or trans. Notably, most ncRNAs do not encode proteins, but some encode small polypeptides. We were also interested in ncRNA, which encodes peptides that add to antiviral innate immunity. Compared to other types of ncRNAs, lncRNAs exhibit surprisingly more functions. However, there are still many unanswered questions, such as whether the evolution of lncRNAs and miRNAs is conserved. In order to solve these outstanding problems, future studies need to focus on lncRNA biology and immune-related lncRNA functions in vivo. In addition, emerging circRNAs are classified as lncRNAs generated by back splicing and 3′ to 5′ end self-ligation. However, few reports address the basic mechanisms of IAV infection and replication, or the regulatory mechanisms by which circRNAs affect the interaction between IAV and host cells. Therefore, research on circRNA with respect to antiviral innate immune responses induced by influenza virus, the molecular basis of virus RNA binding proteins, the circRNA transcription regulatory mechanisms, analysis of circRNA effects on cell function, and determining the network(s) involved in signaling pathways and regulation are worthy of future research. We expect to find that circRNAs regulate cell functions and discover the mechanisms by which they influence viral replication and pathogenicity.
Author Contributions
J.L. conceived and designed the manuscript. J.M. and J.L. prepared the manuscript and completed its revision. W.L. suggested many of the ideas presented in this study. All authors have read and agreed to the published version of the manuscript.
Funding
This work was supported by grants from the National Natural Science Foundation of China (32170143, 32061123001, 31970153). J.L. is supported by the Youth Innovation Promotion Association of CAS (2019091).
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Crick, F. Central dogma of molecular biology. Nature 1970, 227, 561–563. [Google Scholar] [CrossRef] [Scilit]
- Crick, F.H. On protein synthesis. Symp. Soc. Exp. Biol. 1958, 12, 138–163. [Google Scholar] [PubMed]
- Consortium, E.P. An integrated encyclopedia of DNA elements in the human genome. Nature 2012, 489, 57–74. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schneider, W.M.; Chevillotte, M.D.; Rice, C.M. Interferon-stimulated genes: A complex web of host defenses. Annu. Rev. Immunol. 2014, 32, 513–545. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Yang, W.; Wang, X.; Zhang, X.; Tian, H.; Deng, H.; Zhang, L.; Gao, G. Identification of new type I interferon-stimulated genes and investigation of their involvement in IFN-beta activation. Protein Cell 2018, 9, 799–807. [Google Scholar] [CrossRef] [Scilit]
- Der, S.D.; Zhou, A.; Williams, B.R.; Silverman, R.H. Identification of genes differentially regulated by interferon alpha, beta, or gamma using oligonucleotide arrays. Proc. Natl. Acad. Sci. USA 1998, 95, 15623–15628. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Rani, M.R.; Shrock, J.; Appachi, S.; Rudick, R.A.; Williams, B.R.; Ransohoff, R.M. Novel interferon-beta-induced gene expression in peripheral blood cells. J. Leukoc. Biol. 2007, 82, 1353–1360. [Google Scholar] [CrossRef] [Scilit]
- Sarasin-Filipowicz, M.; Oakeley, E.J.; Duong, F.H.; Christen, V.; Terracciano, L.; Filipowicz, W.; Heim, M.H. Interferon signaling and treatment outcome in chronic hepatitis C. Proc. Natl. Acad. Sci. USA 2008, 105, 7034–7039. [Google Scholar] [CrossRef] [Scilit]
- Indraccolo, S.; Pfeffer, U.; Minuzzo, S.; Esposito, G.; Roni, V.; Mandruzzato, S.; Ferrari, N.; Anfosso, L.; Dell’Eva, R.; Noonan, D.M.; et al. Identification of genes selectively regulated by IFNs in endothelial cells. J. Immunol. 2007, 178, 1122–1135. [Google Scholar] [CrossRef] [Scilit]
- de Veer, M.J.; Holko, M.; Frevel, M.; Walker, E.; Der, S.; Paranjape, J.M.; Silverman, R.H.; Williams, B.R. Functional classification of interferon-stimulated genes identified using microarrays. J. Leukoc. Biol. 2001, 69, 912–920. [Google Scholar] [CrossRef] [Scilit]
- Liu, X.; Duan, X.; Holmes, J.A.; Li, W.; Lee, S.H.; Tu, Z.; Zhu, C.; Salloum, S.; Lidofsky, A.; Schaefer, E.A.; et al. A Long Noncoding RNA Regulates Hepatitis C virus Infection Through Interferon Alpha-Inducible Protein 6. Hepatology 2019, 69, 1004–1019. [Google Scholar] [CrossRef] [Scilit]
- Pan, Q.; Zhao, Z.; Liao, Y.; Chiu, S.H.; Wang, S.; Chen, B.; Chen, N.; Chen, Y.; Chen, J.L. Identification of an Interferon-Stimulated Long Noncoding RNA (LncRNA ISR) Involved in Regulation of Influenza A virus Replication. Int. J. Mol. Sci. 2019, 20, 5118. [Google Scholar] [CrossRef] [Scilit]
- Pedersen, I.M.; Cheng, G.; Wieland, S.; Volinia, S.; Croce, C.M.; Chisari, F.V.; David, M. Interferon modulation of cellular microRNAs as an antiviral mechanism. Nature 2007, 449, 919–922. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Schmitt, M.J.; Philippidou, D.; Reinsbach, S.E.; Margue, C.; Wienecke-Baldacchino, A.; Nashan, D.; Behrmann, I.; Kreis, S. Interferon-gamma-induced activation of Signal Transducer and Activator of Transcription 1 (STAT1) up-regulates the tumor suppressing microRNA-29 family in melanoma cells. Cell Commun. Signal. 2012, 10, 41. [Google Scholar] [CrossRef] [Scilit]
- Yang, C.H.; Yue, J.; Fan, M.; Pfeffer, L.M. IFN induces miR-21 through a signal transducer and activator of transcription 3-dependent pathway as a suppressive negative feedback on IFN-induced apoptosis. Cancer Res. 2010, 70, 8108–8116. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kawai, T.; Akira, S. The role of pattern-recognition receptors in innate immunity: Update on Toll-like receptors. Nat. Immunol. 2010, 11, 373–384. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chan, Y.K.; Gack, M.U. RIG-I-like receptor regulation in virus infection and immunity. Curr. Opin. Virol. 2015, 12, 7–14. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, Q.; Sun, L.; Chen, Z.J. Regulation and function of the cGAS-STING pathway of cytosolic DNA sensing. Nat. Immunol. 2016, 17, 1142–1149. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chan, Y.K.; Gack, M.U. Viral evasion of intracellular DNA and RNA sensing. Nat. Rev. Microbiol. 2016, 14, 360–373. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kotenko, S.V.; Gallagher, G.; Baurin, V.V.; Lewis-Antes, A.; Shen, M.; Shah, N.K.; Langer, J.A.; Sheikh, F.; Dickensheets, H.; Donnelly, R.P. IFN-lambdas mediate antiviral protection through a distinct class II cytokine receptor complex. Nat. Immunol. 2003, 4, 69–77. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sheppard, P.; Kindsvogel, W.; Xu, W.; Henderson, K.; Schlutsmeyer, S.; Whitmore, T.E.; Kuestner, R.; Garrigues, U.; Birks, C.; Roraback, J.; et al. IL-28, IL-29 and their class II cytokine receptor IL-28R. Nat. Immunol. 2003, 4, 63–68. [Google Scholar] [CrossRef] [Scilit]
- Prokunina-Olsson, L.; Muchmore, B.; Tang, W.; Pfeiffer, R.M.; Park, H.; Dickensheets, H.; Hergott, D.; Porter-Gill, P.; Mumy, A.; Kohaar, I.; et al. A variant upstream of IFNL3 (IL28B) creating a new interferon gene IFNL4 is associated with impaired clearance of hepatitis C virus. Nat. Genet. 2013, 45, 164–171. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Alspach, E.; Lussier, D.M.; Schreiber, R.D. Interferon gamma and Its Important Roles in Promoting and Inhibiting Spontaneous and Therapeutic Cancer Immunity. Cold Spring Harb. Perspect. Biol. 2019, 11, a028480. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- van Boxel-Dezaire, A.H.; Rani, M.R.; Stark, G.R. Complex modulation of cell type-specific signaling in response to type I interferons. Immunity 2006, 25, 361–372. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Marcello, T.; Grakoui, A.; Barba-Spaeth, G.; Machlin, E.S.; Kotenko, S.V.; MacDonald, M.R.; Rice, C.M. Interferons alpha and lambda inhibit hepatitis C virus replication with distinct signal transduction and gene regulation kinetics. Gastroenterology 2006, 131, 1887–1898. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolen, C.R.; Ding, S.; Robek, M.D.; Kleinstein, S.H. Dynamic expression profiling of type I and type III interferon-stimulated hepatocytes reveals a stable hierarchy of gene expression. Hepatology 2014, 59, 1262–1272. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Galani, I.E.; Koltsida, O.; Andreakos, E. Type III interferons (IFNs): Emerging Master Regulators of Immunity. Adv. Exp. Med. Biol. 2015, 850, 1–15. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Borden, E.C.; Sen, G.C.; Uze, G.; Silverman, R.H.; Ransohoff, R.M.; Foster, G.R.; Stark, G.R. Interferons at age 50: Past, current and future impact on biomedicine. Nat. Rev. Drug Discov. 2007, 6, 975–990. [Google Scholar] [CrossRef] [Scilit]
- Kambara, H.; Niazi, F.; Kostadinova, L.; Moonka, D.K.; Siegel, C.T.; Post, A.B.; Carnero, E.; Barriocanal, M.; Fortes, P.; Anthony, D.D.; et al. Negative regulation of the interferon response by an interferon-induced long non-coding RNA. Nucleic Acids Res. 2014, 42, 10668–10680. [Google Scholar] [CrossRef] [Scilit]
- Josset, L.; Tchitchek, N.; Gralinski, L.E.; Ferris, M.T.; Eisfeld, A.J.; Green, R.R.; Thomas, M.J.; Tisoncik-Go, J.; Schroth, G.P.; Kawaoka, Y.; et al. Annotation of long non-coding RNAs expressed in collaborative cross founder mice in response to respiratory virus infection reveals a new class of interferon-stimulated transcripts. RNA Biol. 2014, 11, 875–890. [Google Scholar] [CrossRef] [Scilit]
- Barriocanal, M.; Carnero, E.; Segura, V.; Fortes, P. Long Non-Coding RNA BST2/BISPR is Induced by IFN and Regulates the Expression of the Antiviral Factor Tetherin. Front. Immunol. 2014, 5, 655. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Carnero, E.; Barriocanal, M.; Segura, V.; Guruceaga, E.; Prior, C.; Borner, K.; Grimm, D.; Fortes, P. Type I Interferon Regulates the Expression of Long Non-Coding RNAs. Front. Immunol. 2014, 5, 548. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sakai, I.; Takeuchi, K.; Yamauchi, H.; Narumi, H.; Fujita, S. Constitutive expression of SOCS3 confers resistance to IFN-alpha in chronic myelogenous leukemia cells. Blood 2002, 100, 2926–2931. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qin, H.; Niyongere, S.A.; Lee, S.J.; Baker, B.J.; Benveniste, E.N. Expression and functional significance of SOCS-1 and SOCS-3 in astrocytes. J. Immunol. 2008, 181, 3167–3176. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Du, H.; Cui, S.; Li, Y.; Yang, G.; Wang, P.; Fikrig, E.; You, F. MiR-221 negatively regulates innate anti-viral response. PLoS ONE 2018, 13, e0200385. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Liu, S.; Sun, X.; Wang, M.; Hou, Y.; Zhan, Y.; Jiang, Y.; Liu, Z.; Cao, X.; Chen, P.; Liu, Z.; et al. A microRNA 221- and 222-mediated feedback loop maintains constitutive activation of NFkappaB and STAT3 in colorectal cancer cells. Gastroenterology 2014, 147, 847–859.e11. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, C.; Han, L.; Zhang, A.; Yang, W.; Zhou, X.; Pu, P.; Du, Y.; Zeng, H.; Kang, C. Global changes of mRNA expression reveals an increased activity of the interferon-induced signal transducer and activator of transcription (STAT) pathway by repression of miR-221/222 in glioblastoma U251 cells. Int. J. Oncol. 2010, 36, 1503–1512. [Google Scholar] [CrossRef] [Scilit]
- Hertzog, P.; Forster, S.; Samarajiwa, S. Systems biology of interferon responses. J. Interferon Cytokine Res. 2011, 31, 5–11. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Perng, Y.C.; Lenschow, D.J. ISG15 in antiviral immunity and beyond. Nat. Rev. Microbiol. 2018, 16, 423–439. [Google Scholar] [CrossRef] [Scilit]
- Farrell, P.J.; Broeze, R.J.; Lengyel, P. Accumulation of an mRNA and protein in interferon-treated Ehrlich ascites tumour cells. Nature 1979, 279, 523–525. [Google Scholar] [CrossRef] [Scilit]
- Zhang, D.; Zhang, D.E. Interferon-stimulated gene 15 and the protein ISGylation system. J. Interferon Cytokine Res. 2011, 31, 119–130. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chai, W.; Li, J.; Shangguan, Q.; Liu, Q.; Li, X.; Qi, D.; Tong, X.; Liu, W.; Ye, X. Lnc-ISG20 Inhibits Influenza A Virus Replication by Enhancing ISG20 Expression. J. Virol. 2018, 92, e00539-18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Li, X.; Guo, G.; Lu, M.; Chai, W.; Li, Y.; Tong, X.; Li, J.; Jia, X.; Liu, W.; Qi, D.; et al. Long Noncoding RNA Lnc-MxA Inhibits Beta Interferon Transcription by Forming RNA-DNA Triplexes at Its Promoter. J. Virol. 2019, 93, e00786-19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kincaid, R.P.; Sullivan, C.S. Virus-encoded microRNAs: An overview and a look to the future. PLoS Pathog. 2012, 8, e1003018. [Google Scholar] [CrossRef] [Scilit]
- Haussecker, D.; Kay, M.A. miR-122 continues to blaze the trail for microRNA therapeutics. Mol. Ther. 2010, 18, 240–242. [Google Scholar] [CrossRef] [Scilit]
- Chen, Y.; Shen, A.; Rider, P.J.; Yu, Y.; Wu, K.; Mu, Y.; Hao, Q.; Liu, Y.; Gong, H.; Zhu, Y.; et al. A liver-specific microRNA binds to a highly conserved RNA sequence of hepatitis B virus and negatively regulates viral gene expression and replication. FASEB J. 2011, 25, 4511–4521. [Google Scholar] [CrossRef] [Scilit]
- Nathans, R.; Chu, C.Y.; Serquina, A.K.; Lu, C.C.; Cao, H.; Rana, T.M. Cellular microRNA and P bodies modulate host-HIV-1 interactions. Mol. Cell 2009, 34, 696–709. [Google Scholar] [CrossRef] [Scilit]
- Kutty, R.K.; Nagineni, C.N.; Samuel, W.; Vijayasarathy, C.; Hooks, J.J.; Redmond, T.M. Inflammatory cytokines regulate microRNA-155 expression in human retinal pigment epithelial cells by activating JAK/STAT pathway. Biochem. Biophys. Res. Commun. 2010, 402, 390–395. [Google Scholar] [CrossRef] [Scilit]
- Liu, Z.; Qin, Q.; Wu, C.; Li, H.; Shou, J.; Yang, Y.; Gu, M.; Ma, C.; Lin, W.; Zou, Y.; et al. Downregulated NDR1 protein kinase inhibits innate immune response by initiating an miR146a-STAT1 feedback loop. Nat. Commun. 2018, 9, 2789. [Google Scholar] [CrossRef] [Scilit]
- Wang, P.; Hou, J.; Lin, L.; Wang, C.; Liu, X.; Li, D.; Ma, F.; Wang, Z.; Cao, X. Inducible microRNA-155 feedback promotes type I IFN signaling in antiviral innate immunity by targeting suppressor of cytokine signaling 1. J. Immunol. 2010, 185, 6226–6233. [Google Scholar] [CrossRef] [Scilit]
- Zheng, X.-Y.; Bian, P.-Y.; Ye, C.-T.; Ye, W.; Ma, H.-W.; Tang, K.; Zhang, C.-M.; Lei, Y.-F.; Wei, X.; Wang, P.-Z. Interferon-Induced Transmembrane Protein 3 Inhibits Hantaan Virus Infection, and Its Single Nucleotide Polymorphism rs12252 Influences the Severity of Hemorrhagic Fever with Re-nal Syndrome. Front. Immunol. 2016, 7, 535. [Google Scholar]
- Mariotti, B.; Servaas, N.H.; Rossato, M.; Tamassia, N.; Cassatella, M.A.; Cossu, M.; Beretta, L.; van der Kroef, M.; Radstake, T.; Bazzoni, F. The Long Non-coding RNA NRIR Drives IFN-Response in Monocytes: Implication for Systemic Sclerosis. Front. Immunol. 2019, 10, 100. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Paliwal, D.; Joshi, P.; Panda, S.K. Hepatitis E virus (HEV) egress: Role of BST2 (Tetherin) and interferon induced long non- coding RNA (lncRNA) BISPR. PLoS ONE 2017, 12, e0187334. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Carnero, E.; Barriocanal, M.; Prior, C.; Pablo Unfried, J.; Segura, V.; Guruceaga, E.; Enguita, M.; Smerdou, C.; Gastaminza, P.; Fortes, P. Long noncoding RNA EGOT negatively affects the antiviral response and favors HCV replication. EMBO Rep. 2016, 17, 1013–1028. [Google Scholar] [CrossRef] [Scilit]
- Nishitsuji, H.; Ujino, S.; Yoshio, S.; Sugiyama, M.; Mizokami, M.; Kanto, T.; Shimotohno, K. Long noncoding RNA #32 con-tributes to antiviral responses by controlling interferon-stimulated gene expression. Proc. Natl. Acad. Sci. USA 2016, 113, 10388–10393. [Google Scholar]
- Xie, Q.; Chen, S.; Tian, R.; Huang, X.; Deng, R.; Xue, B.; Qin, Y.; Xu, Y.; Wang, J.; Guo, M.; et al. Long Noncoding RNA ITPRIP-1 Positively Regulates the Innate Immune Response through Promotion of Oligomerization and Activation of MDA5. J. Virol. 2018, 92, e00507-18. [Google Scholar] [CrossRef] [Scilit]
- Zhou, Y.; Li, M.; Xue, Y.; Li, Z.; Wen, W.; Liu, X.; Ma, Y.; Zhang, L.; Shen, Z.; Cao, X. Interferon-inducible cytoplasmic lncLrrc55-AS promotes antiviral innate responses by strengthening IRF3 phosphorylation. Cell Res. 2019, 29, 641–654. [Google Scholar] [CrossRef] [Scilit]
- Jiang, M.; Zhang, S.; Yang, Z.; Lin, H.; Zhu, J.; Liu, L.; Wang, W.; Liu, S.; Liu, W.; Ma, Y.; et al. Self-Recognition of an Inducible Host lncRNA by RIG-I Feedback Restricts Innate Immune Response. Cell 2018, 173, 906–919.e13. [Google Scholar] [CrossRef] [Scilit]
- More, S.; Zhu, Z.; Lin, K.; Huang, C.; Pushparaj, S.; Liang, Y.; Sathiaseelan, R.; Yang, X.; Liu, L. Long non-coding RNA PSMB8-AS1 regulates influenza virus replication. RNA Biol. 2019, 16, 340–353. [Google Scholar] [CrossRef] [Scilit]
- Kambara, H.; Gunawardane, L.; Zebrowski, E.; Kostadinova, L.; Jobava, R.; Krokowski, D.; Hatzoglou, M.; Anthony, D.D.; Valad-khan, S. Regulation of Interferon-Stimulated Gene BST2 by a lncRNA Transcribed from a Shared Bidirectional Pro-moter. Front. Immunol. 2014, 5, 676. [Google Scholar]
- Perez-Caballero, D.; Zang, T.; Ebrahimi, A.; McNatt, M.W.; Gregory, D.A.; Johnson, M.C.; Bieniasz, P.D. Tetherin inhibits HIV-1 release by directly tethering virions to cells. Cell 2009, 139, 499–511. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mangeat, B.; Cavagliotti, L.; Lehmann, M.; Gers-Huber, G.; Kaur, I.; Thomas, Y.; Kaiser, L.; Piguet, V. Influenza virus partially counteracts restriction imposed by tetherin/BST-2. J. Biol. Chem. 2012, 287, 22015–22029. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Gao, S.; von der Malsburg, A.; Paeschke, S.; Behlke, J.; Haller, O.; Kochs, G.; Daumke, O. Structural basis of oligomerization in the stalk region of dynamin-like MxA. Nature 2010, 465, 502–506. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kane, M.; Yadav, S.S.; Bitzegeio, J.; Kutluay, S.B.; Zang, T.; Wilson, S.J.; Schoggins, J.W.; Rice, C.M.; Yamashita, M.; Hatziioannou, T.; et al. MX2 is an interferon-induced inhibitor of HIV-1 infection. Nature 2013, 502, 563–566. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Goujon, C.; Moncorge, O.; Bauby, H.; Doyle, T.; Ward, C.C.; Schaller, T.; Hue, S.; Barclay, W.S.; Schulz, R.; Malim, M.H. Human MX2 is an interferon-induced post-entry inhibitor of HIV-1 infection. Nature 2013, 502, 559–562. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zimmermann, P.; Manz, B.; Haller, O.; Schwemmle, M.; Kochs, G. The viral nucleoprotein determines Mx sensitivity of influenza A viruses. J. Virol. 2011, 85, 8133–8140. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, X.; Yan, Y.; Lin, W.; Li, A.; Zhang, H.; Lei, X.; Dai, Z.; Li, X.; Li, H.; Chen, W.; et al. Circular RNA Vav3 sponges gga-miR-375 to promote epithelial-mesenchymal transition. RNA Biol. 2019, 16, 118–132. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tagawa, T.; Gao, S.; Koparde, V.N.; Gonzalez, M.; Spouge, J.L.; Serquina, A.P.; Lurain, K.; Ramaswami, R.; Uldrick, T.S.; Yarchoan, R.; et al. Discovery of Kaposi’s sarcoma herpesvirus-encoded circular RNAs and a human antiviral circular RNA. Proc. Natl. Acad. Sci. USA 2018, 115, 12805–12810. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhao, J.; Lee, E.E.; Kim, J.; Yang, R.; Chamseddin, B.; Ni, C.; Gusho, E.; Xie, Y.; Chiang, C.M.; Buszczak, M.; et al. Transforming activity of an oncoprotein-encoding circular RNA from human papillomavirus. Nat. Commun. 2019, 10, 2300. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Yu, T.; Ding, Y.; Zhang, Y.; Liu, Y.; Li, Y.; Lei, J.; Zhou, J.; Song, S.; Hu, B. Circular RNA GATAD2A promotes H1N1 replication through inhibiting autophagy. Vet. Microbiol. 2019, 231, 238–245. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, Y.G.; Kim, M.V.; Chen, X.; Batista, P.J.; Aoyama, S.; Wilusz, J.E.; Iwasaki, A.; Chang, H.Y. Sensing Self and Foreign Circular RNAs by Intron Identity. Mol. Cell 2017, 67, 228–238.e5. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Glazar, P.; Papavasileiou, P.; Rajewsky, N. circBase: A database for circular RNAs. RNA 2014, 20, 1666–1670. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Qu, Z.; Meng, F.; Shi, J.; Deng, G.; Zeng, X.; Ge, J.; Li, Y.; Liu, L.; Chen, P.; Jiang, Y.; et al. A Novel Intronic Circular RNA Antagonizes Influenza virus by Absorbing a microRNA That Degrades CREBBP and Accelerating IFN-beta Production. mBio 2021, 12, e0101721. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Guo, Y.; Yu, X.; Su, N.; Shi, N.; Zhang, S.; Zhang, L.; Yang, L.; Zhao, L.; Guan, Z.; Zhang, M.; et al. Identification and characterization of circular RNAs in the A549 cells following Influenza A virus infection. Vet. Microbiol. 2022, 267, 109390. [Google Scholar] [CrossRef] [Scilit]
- Zhang, Y.; Zhang, Y.; Li, X.; Zhang, M.; Lv, K. Microarray analysis of circular RNA expression patterns in polarized macrophages. Int. J. Mol. Med. 2017, 39, 373–379. [Google Scholar] [CrossRef] [Scilit]
- Iyer, M.K.; Niknafs, Y.S.; Malik, R.; Singhal, U.; Sahu, A.; Hosono, Y.; Barrette, T.R.; Prensner, J.R.; Evans, J.R.; Zhao, S.; et al. The landscape of long noncoding RNAs in the human transcriptome. Nat. Genet. 2015, 47, 199–208. [Google Scholar] [CrossRef] [Scilit]
- Peng, X.; Gralinski, L.; Armour, C.D.; Ferris, M.T.; Thomas, M.J.; Proll, S.; Bradel-Tretheway, B.G.; Korth, M.J.; Castle, J.C.; Biery, M.C.; et al. Unique signatures of long noncoding RNA expression in response to virus infection and altered innate immune signaling. mBio 2010, 1, e00206-10. [Google Scholar] [CrossRef] [Scilit]
- Laha, S.; Saha, C.; Dutta, S.; Basu, M.; Chatterjee, R.; Ghosh, S.; Bhattacharyya, N.P. In silico analysis of altered expression of long non-coding RNA in SARS-CoV-2 infected cells and their possible regulation by STAT1, STAT3 and interferon regulatory factors. Heliyon 2021, 7, e06395. [Google Scholar] [CrossRef] [Scilit]
- Shaw, A.E.; Hughes, J.; Gu, Q.; Behdenna, A.; Singer, J.B.; Dennis, T.; Orton, R.J.; Varela, M.; Gifford, R.J.; Wilson, S.J.; et al. Fundamental properties of the mammalian innate immune system revealed by multispecies comparison of type I interferon responses. PLoS Biol. 2017, 15, e2004086. [Google Scholar] [CrossRef] [Scilit]
- Sen, G.C.; Sarkar, S.N. The interferon-stimulated genes: Targets of direct signaling by interferons, double-stranded RNA, and viruses. Curr. Top. Microbiol. Immunol. 2007, 316, 233–250. [Google Scholar] [CrossRef] [Scilit]
- Lew, D.J.; Decker, T.; Darnell, J.E., Jr. Alpha interferon and gamma interferon stimulate transcription of a single gene through different signal transduction pathways. Mol. Cell. Biol. 1989, 9, 5404–5411. [Google Scholar] [CrossRef] [Scilit]
- Fenner, J.E.; Starr, R.; Cornish, A.L.; Zhang, J.G.; Metcalf, D.; Schreiber, R.D.; Sheehan, K.; Hilton, D.J.; Alexander, W.S.; Hertzog, P.J. Suppressor of cytokine signaling 1 regulates the immune response to infection by a unique inhibition of type I interferon activity. Nat. Immunol. 2006, 7, 33–39. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Winterling, C.; Koch, M.; Koeppel, M.; Garcia-Alcalde, F.; Karlas, A.; Meyer, T.F. Evidence for a crucial role of a host non-coding RNA in influenza A virus replication. RNA Biol. 2014, 11, 66–75. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Budhiraja, S.; Liu, H.; Couturier, J.; Malovannaya, A.; Qin, J.; Lewis, D.E.; Rice, A.P. Mining the human complexome database identifies RBM14 as an XPO1-associated protein involved in HIV-1 Rev function. J. Virol. 2015, 89, 3557–3567. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Zhang, Q.; Chen, C.Y.; Yedavalli, V.S.; Jeang, K.T. NEAT1 long noncoding RNA and paraspeckle bodies modulate HIV-1 posttranscriptional expression. mBio 2013, 4, e00596-12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Imamura, K.; Imamachi, N.; Akizuki, G.; Kumakura, M.; Kawaguchi, A.; Nagata, K.; Kato, A.; Kawaguchi, Y.; Sato, H.; Yoneda, M.; et al. Long noncoding RNA NEAT1-dependent SFPQ relocation from promoter region to paraspeckle mediates IL8 expression upon immune stimuli. Mol. Cell 2014, 53, 393–406. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wang, Z.; Fan, P.; Zhao, Y.; Zhang, S.; Lu, J.; Xie, W.; Jiang, Y.; Lei, F.; Xu, N.; Zhang, Y. NEAT1 modulates herpes simplex virus-1 replication by regulating viral gene transcription. Cell. Mol. Life Sci. 2017, 74, 1117–1131. [Google Scholar] [CrossRef] [Scilit]
- Ma, H.; Han, P.; Ye, W.; Chen, H.; Zheng, X.; Cheng, L.; Zhang, L.; Yu, L.; Wu, X.; Xu, Z.; et al. The Long Noncoding RNA NEAT1 Exerts Antihantaviral Effects by Acting as Positive Feedback for RIG-I Signaling. J. Virol. 2017, 91, e02250-16. [Google Scholar] [CrossRef] [Scilit]
- Beeharry, Y.; Goodrum, G.; Imperiale, C.J.; Pelchat, M. The Hepatitis Delta virus accumulation requires paraspeckle components and affects NEAT1 level and PSP1 localization. Sci. Rep. 2018, 8, 6031. [Google Scholar] [CrossRef] [Scilit]
- Pandey, A.D.; Goswami, S.; Shukla, S.; Das, S.; Ghosal, S.; Pal, M.; Bandyopadhyay, B.; Ramachandran, V.; Basu, N.; Sood, V.; et al. Correlation of altered expression of a long non-coding RNA, NEAT1, in peripheral blood mononuclear cells with dengue disease progression. J. Infect. 2017, 75, 541–554. [Google Scholar] [CrossRef] [Scilit]
- Nombela, P.; Miguel-Lopez, B.; Blanco, S. The role of m(6)A, m(5)C and Psi RNA modifications in cancer: Novel therapeutic opportunities. Mol. Cancer 2021, 20, 18. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kong, S.; Tao, M.; Shen, X.; Ju, S. Translatable circRNAs and lncRNAs: Driving mechanisms and functions of their translation products. Cancer Lett. 2020, 483, 59–65. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2022 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).