


Abstract
Spirulina microalgae contain a plethora of nutrient and non-nutrient molecules providing brain health benefits. Numerous in vivo evidence has provided support for the brain health potential of spirulina, highlighting antioxidant, anti-inflammatory, and neuroprotective mechanisms. Preliminary clinical studies have also suggested that spirulina can help to reduce mental fatigue, protect the vascular wall of brain vessels from endothelial damage and regulate internal pressure, thus contributing to the prevention and/or mitigating of cerebrovascular conditions. Furthermore, the use of spirulina in malnourished children appears to ameliorate motor, language, and cognitive skills, suggesting a reinforcing role in developmental mechanisms. Evidence of the central effect of spirulina on appetite regulation has also been shown. This review aims to understand the applicative potential of spirulina microalgae in the prevention and mitigation of brain disorders, highlighting the nutritional value of this “superfood”, and providing the current knowledge on relevant molecular mechanisms in the brain associated with its dietary introduction.
1. Introduction
The brain is the body’s central control center for most physiological activities processing, integrating, and coordinating the information from peripheral sense organs, and responding with centrally elaborated instructions appropriately conveyed back to the periphery in each area of the body [1]. Keeping a healthy brain is thus fundamental to maintaining a correct function in every aspect of physiological, psychological, and social life. Following a healthy lifestyle and providing dietary nutrients and non-nutrient molecules can help to prevent or mitigate brain disorders that in turn, can affect the entire body’s functions [1,2]. Brain disorders include several conditions or disabilities that affect the brain and are caused by degenerative diseases, mental illnesses, and genetic or traumatic injuries [2]. It is known how diet can contribute to and influence the development of several neurodegenerative and mental diseases, in particular the lack of specific molecules essential for the brain [2]. Proper dietary factors can contribute to maintaining neuronal functions and synaptic plasticity, through the activation of pivotal biological mechanisms underlying brain health and mental functions. For instance, a diet rich in omega 3, choline, magnesium, B vitamins and vitamin D, specific amino acids, and phytoderivates derived from plants or seaweeds, among others, can promote brain health and preserve mental functions while reducing the onset of neurodegenerative and mental diseases [2,3].
Seaweeds provide a vast series of micro- and macronutrients (e.g., B vitamins, minerals, amino acids, etc.) and phytochemical compounds relevant for brain health. When included in the diet, they first interact with the microbiome residing in the gastrointestinal tract [4,5]. Seaweed–microbiota interaction can lead to the production of small bioactive molecules, which can affect intestinal ecology and subsequently host brain health by growth-promoting (prebiotic) effects of specific bacterial genera involved in the production of neurotransmitters, such as GABA and serotonin [4,6]. Experimental evidence has shown that bioactive seaweed-derivatives can reach and enter the brain and modulate multiple neuronal functions both directly, through specific neuronal molecules and antioxidant and anti-inflammatory activity, and indirectly by epigenetic mechanisms affecting the transcription of proteins involved in neurotransmissions, neuronal survival, and plasticity [7,8,9,10,11,12,13].
Studies on human subjects are increasingly associating seaweeds with neuroprotective and cognitive-enhancing actions. This includes Ulva lactuca, Laminaria japonica, Ascophyllum nodosum, Fucus vesiculosus, and Spirulina spp. [14,15,16]. In particular, Spirulina spp., given their high content of amino acids, vitamins, minerals, and a peculiar phytocomplex, are currently under investigation for their potential neuroprotective and cognitive-enhancing functions [17].
This review focuses on the beneficial effects of spirulina microalgae in the prevention or mitigation of brain disorders by analyzing the potential neuroprotective molecular mechanisms highlighted in current experimental data in vitro and in vivo studies, as well as in preliminary clinical observations that seem to encourage the use of spirulina for brain health.
2. Spirulina Microalgae: Sources, Chemical Composition, and Bioavailability
Spirulina (Arthrospira platensis (Nordstedt) Gomont, or Spirulina platensis) is a species belonging to the Cyanobacteria class (cyanobacteria) that lives in freshwater lakes with alkaline and warm waters (e.g., Lake Texcoco, Lake Chad, etc.) [11,18]. Along with Spirulina platensis, another commonly used species of spirulina for food supplements is Spirulina maxima [19,20]. Both species have a long history of use as food and can grow in many places worldwide thanks to an astonishing ability to thrive in climatic conditions that are adverse to other algae’s growth. Today, the main growing habitats of spirulina are the Pacific Ocean near Japan and Hawaii, and large freshwater lakes, including Lake Chad in Africa, Lake Klamath in North America, Lake Texcoco in Mexico, and Lake Titicaca in South America. Nowadays, spirulina’s world production as a food supplement is mainly in special algal farms in outdoor tanks and bioreactors [21]. The United States leads the world’s production, followed by Thailand, India, Japan, and China. The nutrient content varies considerably and depends on the production area, the climate, and the water’s salinity in which the algae grow. Harvesting procedures can also influence the content of vitamins, minerals, and phytoderivatives. Furthermore, production processes should always guarantee the absence of heavy metals that can quickly accumulate in the algae [18,21].
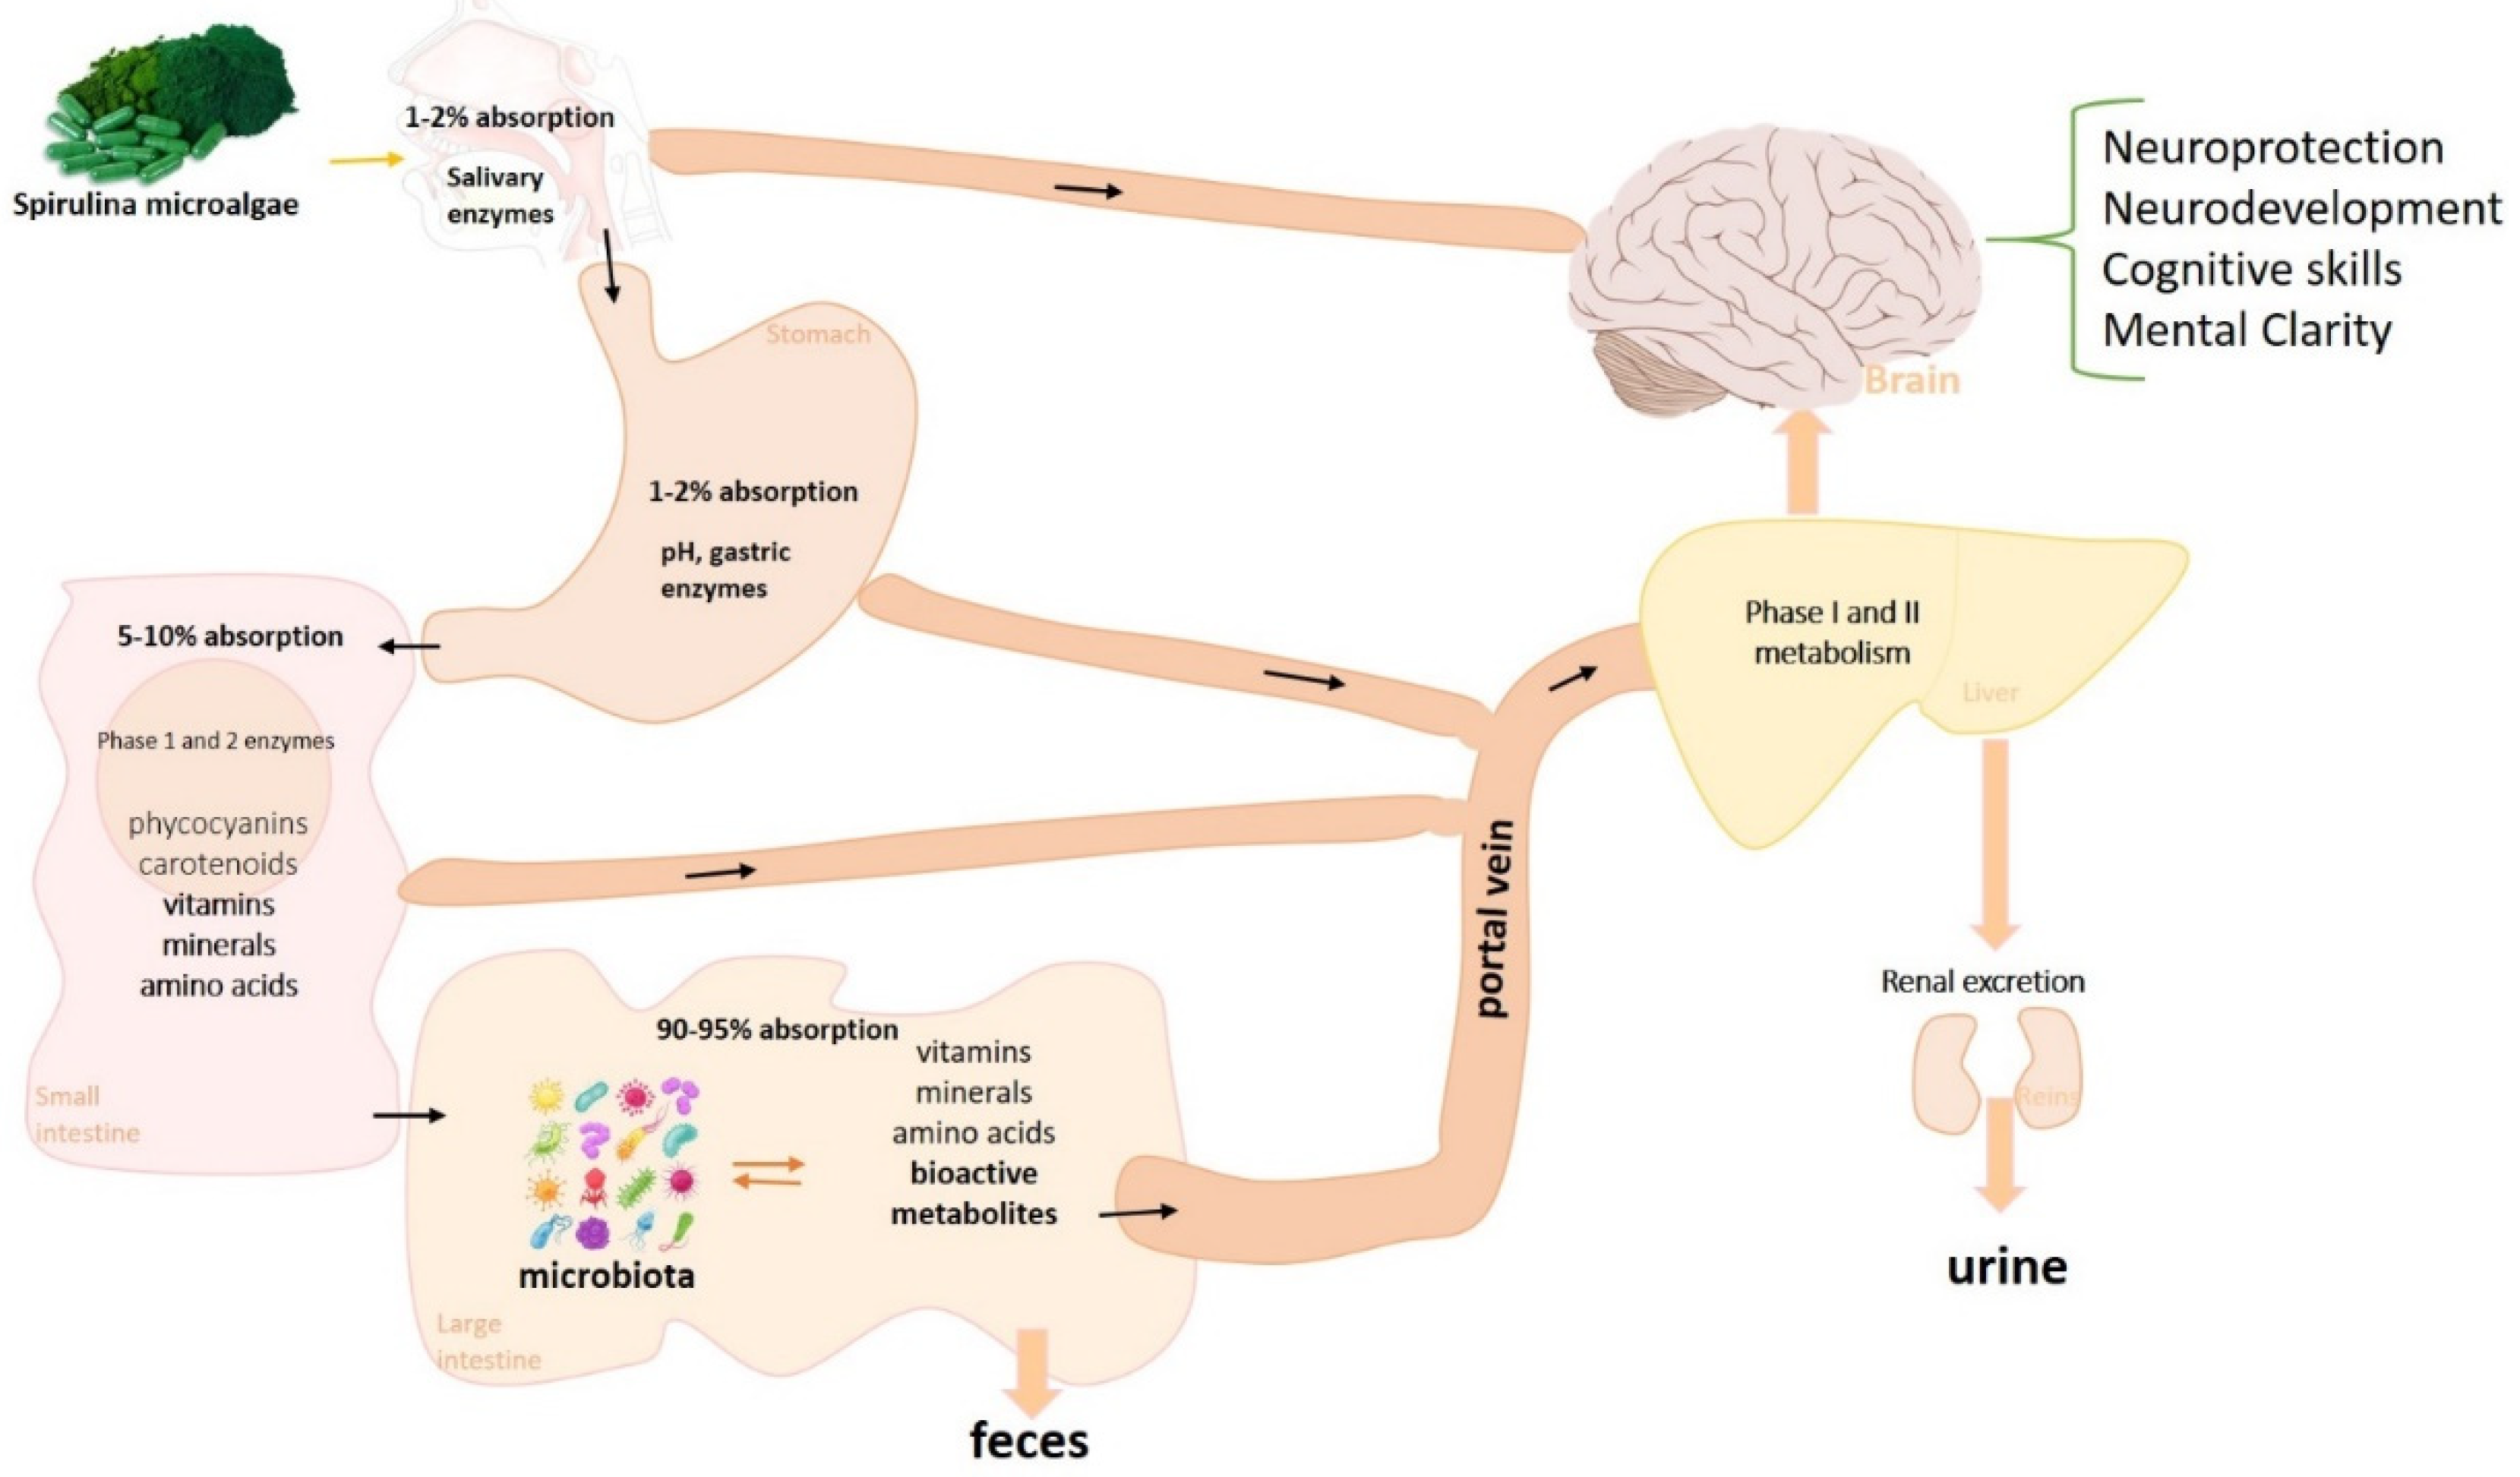
Spirulina species have a significant content of proteins, essential amino acids, vitamins, carotenoids, minerals, essential fatty acids, polysaccharides, glycolipids, etc. [22,23,24], and for this reason, they are commonly used as functional foods whose consumption benefits human health and improves physical and mental performance [18]. The WHO pointed out that spirulina is one of the most relevant superfoods on earth, and NASA uses it for space travel, thanks to the wide range of nutrients that a small amount can provide [25]. In fact, spirulina contains a high level of B vitamins, in particular vitamin B12, and minerals including iron, calcium, zinc, magnesium, manganese, and potassium [26]. In addition, some essential fatty acids, such as gamma-linolenic acid (GLA) are present. Its phytocomplex is instead rich in pigments, including chlorophyll, phycobilins such as phycocyanin, and allophycocyanin (Table 1) [22,27,28]. It is important to note that spirulina nutrients are readily absorbed by the body and quickly restore deficient nutritional status to physiological levels [27]. In particular, the high bioavailability of micronutrients allows their rapid distribution even in the nervous system. B vitamins, magnesium, and fatty acids easily reach the brain through specific carriers exerting beneficial neuronal effects [26,28]. Moreover, as for other phytoderivates [29,30], spirulina phytocomplex can also affect the brain through a first interaction with the intestinal microbiota. In fact, preliminary in vivo evidence currently shows a bidirectional interaction between spirulina and the gut microbiota. On the one hand, the microbiota can biotransform the spirulina phytocomplex into small bioactive molecules able to reach the blood and exert their beneficial functions; on the other hand, spirulina seems to modulate the microbiota diversity towards an increase in the relative abundance of protective bacteria (Figure 1) [31,32].
Figure 1.
Putative absorption, metabolism, and distribution in the CNS of spirulina nutrients and phyto-derivatives. Spirulina microalgae contain a plethora of nutrient molecules and phyto-derivatives which, once taken orally, can follow different ways of absorption. In particular, most of the nutrients such as minerals, vitamins, and amino acids are rapidly absorbed through specific transporters present in the colon and duodenum although a small part can also be absorbed at the sublingual level and in the stomach. The phyto-derivatives, on the other hand, mainly undergo metabolism by phase 1 and 2 enzymes residing in the small intestine despite the majority of phytoderivates metabolism taking place in the duodenum by the intestinal microbiota that biotransforms the phyto-derivatives into small bioactive metabolites able to enter the bloodstream [31,32,33,34].
In particular, the influence of the intestinal microbiota on the central and autonomic nervous system can explain the neuroprotective role of spirulina. In a striking example of trans-kingdom symbiosis, gut microbiota cooperates with their human hosts to coordinate the development and function of the nervous systems through dynamic bidirectional communication along the so-called gut–brain axis [33]. Disruptions in microbial communities have been implicated in several neurological disorders and the use of probiotic and prebiotic compounds, such as those in the spirulina phytocomplex, can preserve gut microbiota homeostasis and prevent the development of brain disorders [34].
Recent in vivo studies demonstrate that oral administration of spirulina once daily for 24 consecutive days altered the diversity, structure, and composition of the colonic microbial community at the genus level, including the relative abundance of Clostridium XIVa, Desulfovibrio, Eubacterium, Barnesiella, and Bacteroides, highlighting a dose-related modulation of the intestinal microbiota and physiological states by spirulina, which can be considered as a potential source of prebiotics for beneficial health effects through interaction with the intestinal microbiota [32]. Yu et al. also demonstrated a microbiota-effect of Spirulina platensis on the relative amount of Proteobacteria and the Firmicutes/Bacteroidetes ratio in fecal samples from rats fed with HFD [35].
By maintaining microbial homeostasis by reducing Proteobacteria hyperproliferation, favoring short-chain fatty acids (SCFA) production and keeping an intestinal barrier integrity, spirulina allows to reduce systemic inflammatory responses which can affect the brain health. A recent study investigated the effects of different doses of phycocyanin, one of the most common pigments in spirulina, on the gut microbiota and gut barrier integrity in mice. The results highlighted an increase in the saccharolytic bacteria of the Lachnospiraceae and Ruminococcaceae families, which can produce butyric acid, and an increase in the Rikenellaceae family, which contains hydrogen-producing bacteria. Furthermore, phycocyanin treatment reduced intestinal permeability and increased intestinal barrier function [36].
The modulation of microbiota diversity is, thus, one of the potential mechanisms of action of spirulina. The impact of spirulina microalgae on the gut microbiota homeostasis should be deeply analyzed by further in vivo studies to understand its mechanism of action at the CNS.
Human studies must expand these preliminary results as the gut microbiota’s effect on the bioavailability and biotransformation of spirulina could be crucial for understanding its actions on energy metabolism, appetite regulation, and brain health.
Table 1.
Nutrients and Phytoderivates of spirulina microalgae relevant for brain health.
3. Spirulina and Brain Health: In Vivo Evidence and Related Mechanism of Action
Many in vivo studies on different animal models using spirulina have highlighted several neuroprotective effects in different brain areas. Table 2 shows the main in vivo studies that have associated the use of spirulina with a neuroprotective effect. Experimental models have been used to test neuroprotection in various circumstances, from neuroinflammation to neurodegeneration, neurotoxicity, and more. One of the earliest pieces of evidence of neuroprotection in vivo was obtained in a neuroinflammation model. In particular, spirulina administration was found to reduce the acute systemic inflammatory insult of lipopolysaccharide (LPS) in young rats, which led to a decline in neural stem cell proliferation. Indeed, a spirulina dietary supplementation was found to significantly protect the proliferative potential of hippocampal neural progenitor cells [45]. The neuroprotective effect of spirulina from neuroinflammatory insults was further confirmed in an LPS-treated rat pups model where spirulina was administered to lactating mothers. In this case, LPS-induced inflammatory IL-1β was reduced, while the LPS-induced inhibition of the expression of antioxidant γglutamylcysteine ligase catalytic subunit (γGCLC), Nrf2, brain-derived neurotrophic factor (BDNF) was reversed, possibly via normalizing effects on phosphorylated AKT (pAKT) [46]. This result was further confirmed later in a similar model. Spirulina dietary supplementation to lactating mothers was confirmed to be able to protect against LPS-induced neuroinflammation in particular by reversing the decreased antioxidant defense in the brain following inflammation, an effect associated with decreased levels of phosphorylated p38 and an increase in the anti-oxidant miRNA 146a [47]. Spirulina has been shown also to exert neuroprotective effects in experimental models of neurodegenerative diseases. In a mouse model of Alzheimer’s disease, treatment with spirulina platensis water extract was suggested to prevent loss of memory by a reduction in the deposition of the amyloid β-protein in the brain, as well as by the increase in the antioxidant activity of glutathione peroxidase and the catalase activity [49]. In a different model where a cognitive disorder was induced in mice by amyloid β 1–42 icv injection, treatment with ethanol extract of spirulina maxima ameliorated cognitive impairments by inhibiting the increased phosphorylation of glycogen synthase kinase-3 and increased glutathione and activating the BDNF/phosphatidylinositol-3 kinase/serine/threonine-protein kinase signaling pathway [50]. The anti-inflammatory/anti-oxidant properties of spirulina have been also studied in Parkinson’s disease (PD) models. In a rat α-Synuclein PD model where neurodegeneration is at least partially mediated by microglial activation, spirulina administration was shown to be neuroprotective [51]. Spirulina platensis was also shown to be neuroprotective in a 6OHDA PD rat model, both in the behavioral test and in neuronal survival, an effect possibly associated with a decrease in the inflammatory enzymes iNOS and COX-2 [52]. Spirulina maxima extract was also shown to ameliorate scopolamine-induced dementia in mice, demonstrated in the Morris water maze and passive avoidance tests. The effect was associated with the increased phosphorylation of both extracellular signal-regulated kinase (p-ERK) and p-cAMP response element-binding protein (p-CREB) as well as the increase in BDNF [53]. Neuroprotective activity by spirulina in neurodegeneration has also been shown in other in vivo models and has been suggested to be mediated by an antioxidant activity associated with the increase of superoxide dismutase, catalase, and glutathione peroxidase [54]. Models of neurotoxicity have also been used to demonstrate spirulina neuroprotection. Neurotoxicity in newborn rats due to prenatal exposure to lead acetate on brain tissues could be strongly alleviated when mothers were fed with spirulina, an effect associated with the reversal of the lead-induced oxidative stress and changes in antioxidant enzyme activities in brain tissues [55]. Similarly, spirulina platensis co-administration was shown to reverse the oxidative damage induced by acute lead acetate administration to rats. An effect that was demonstrated to be mediated by the induction of caspase 3 gene expression in a similar rat model of lead-induced neurotoxicity, using spirulina maxima [56]. Spirulina platensis also demonstrated a neuroprotective activity in other neurotoxic paradigms, in particular in sodium fluoride and manganese treated animals, always associating the protective activity to an antioxidant effect [57,58]. The neuroprotective antioxidant activity of spirulina has also been demonstrated more directly in models of cerebral ischemia-reperfusion injury in rats. Pretreatment with spirulina significantly reduced the experimental neurological deficits and restored the decreased superoxide dismutase (SOD, glutathione (GSH) and catalase (CAT), indicating a clear association with antioxidant enzymatic activity [59]. Other experimental models of neuronal protection have provided further evidence of spirulina antioxidant and anti-inflammatory activity in the brain [60,61,62,63,64,65].
Table 2.
Effects of spirulina in brain health: in vivo evidence.
Taken together these data show that Spirulina spp. can indeed exert neuroprotection by inhibiting/reversing both inflammatory and oxidative neurotoxic mechanisms at several molecular levels in the brain.
4. Spirulina and Brain Health: Potential Clinical Application
Marine algae are considered a food source with unique active ingredients and potential health benefits. The antioxidant, anti-inflammatory, cholesterol homeostasis regulation, protein clearance, and anti-amyloidogenic properties confirm effective protection against oxidative stress, neuroinflammation, and mitochondrial dysfunction which are known to be implicated in the pathophysiology of neurodegenerative disorders and complications associated with cerebral ischemic events and other brain injuries. Algal compounds have been observed in various preclinical studies to confer neuroprotection against a wide range of neurotoxic stressors, such as oxygen/glucose deprivation, hydrogen peroxide, glutamate, β amyloid, or 1-methyl-4-phenylpyridinium (MPP+) and, therefore, are promising therapeutic products for brain disorders (Table 3). Numerous algal compounds with promising neuroprotective capabilities have been identified but only a few have been used in clinical trials. The approval of an algal oligosaccharide, sodium oligomannate, for the treatment of Alzheimer’s disease has recently been approved, which could guide the discovery of seaweed-based drugs [17].
In a randomized, double-blind, placebo-controlled study, the antioxidant capacity, immunomodulatory and lipid-lowering effects of spirulina administered at a dose of 8 g/day for 16 consecutive weeks in healthy elderly subjects were evaluated. In this study, a significant reduction in total plasma cholesterol levels, a significant increase in plasma interleukin IL-2 concentration and IL-6 concentration, and a significant increase in superoxide dismutase activity after supplementation were observed, demonstrating that spirulina has favorable effects on the lipid profile, on the immune system and the antioxidant capacity of elderly subjects, becoming a useful functional food [67].
Spirulina has also been shown to be able to increase people’s ability to resist mental and physical fatigue. In a randomized, double-blind, placebo-controlled study, spirulina supplementation at a dose of 3 g/day after 1 week produced a small, but statistically significant increase in exercise stamina and improved cognitive performance in as little as 4 h after the first supplementation [68]. In another randomized, double-blind clinical trial, it was observed that Arthrospira (spirulina) supplementation of 4.5 g per day, with or without an aerobic exercise program alternating with high-intensity interval training, was associated with significant reductions in all plasma lipids (decrease in total cholesterol, triglyceride, and LDL cholesterol levels and an increase in HDL cholesterol), with a decrease in the Body Mass Index [69]. In a randomized longitudinal study conducted in infants and children from Zambia, it was observed that a 16-month supplementation of spirulina improved the children’s motor development, language, and personal and social skills [70].
Beneficial effects of spirulina have also been found on blood glucose, lipids, and blood pressure levels. In a randomized, double-blind, placebo-controlled study, patients with hypertension but free from other cardiovascular diseases, after 3 months of supplementation with 2.0 g Hawaiian spirulina, showed a significant reduction in systolic blood pressure and body mass index, and an improvement of endothelial function [71]. Similar results were also obtained in another study in which Spirulina platensis was administered at a dose of 1 g per day for 12 weeks. This study found a decrease in total cholesterol levels and an increase in the serum concentration of HDL cholesterol, helping to control and prevent obesity-related disorders [72].
Spirulina maxima have shown beneficial effects not only as an antidyslipidemic but also as an antioxidant and antihypertensive. In a randomized clinical trial, it was observed that after administration of 4.5 g of Spirulina maxima for 12 weeks in patients with arterial hypertension there were statistically significant reductions in systolic blood pressure and levels of sVCAM-1, sE-selectin, and endothelin-1, and an increase in glutathione peroxidase activity [73].
In a double-blind, randomized, placebo-controlled clinical trial, it was found that the intake of a brown seaweed extract improved cognitive functions, in particular episodic memory and attention, in the postprandial phase and associated these effects with optimization of blood glucose levels and insulin response [16].
The identification of phytocomplexes worthy of being studied in clinical trials requires modern approaches, such as virtual screening and systems biology [74], to strengthen the development process of algae-based drugs. Computational studies could provide some crucial information on the ADME properties of potential active ingredients or phytocomplexes, and the molecular docking studies could intercept their interactions and binding affinities with molecular targets [75]. The results obtained through a systems biology approach will allow to identify potential interactions with target molecules and cell signaling pathways at the systemic level. With the constant discovery of new compounds, all of these strategies will accelerate the design and development of future algae-based drugs.
Table 3.
Direct and indirect clinical application of spirulina microalgae on brain health.
5. Conclusions and Future Perspectives
Spirulina microalgae represent a source of nutrients and a phytocomplex that, taken with diet or through regulated supplementation, can support normal brain functions and the development of the nervous system, compensating for nutritional deficiencies such as those frequently encountered in developing countries. Various in vivo evidence testify to peculiar mechanisms of neuroprotection and appetite regulation, as well as antioxidant and anti-inflammatory mechanisms in the brain parenchyma with potential uses in the prevention of neurodegenerative or psychocognitive pathologies, where the inflammatory component is relevant. Preliminary clinical studies are suggesting a neuroprotective role for spirulina supplementation, especially in malnourished children, by enhancing brain development, and motor and language skills. Moreover, spirulina has been shown to improve mental and physical fatigue, probably thanks to its high levels of various brain nutrients (Table 1). Interestingly, blood pressure regulation by spirulina microalgae has been associated with stroke prevention. Despite numerous and encouraging preclinical studies, as well as some initial clinical evidence, additional clinical studies are needed to further clarify the neuroprotective actions of spirulina microalgae.
Author Contributions
All authors wrote the manuscript. All authors have read and agreed to the published version of the manuscript.
Funding
This research received no external funding.
Institutional Review Board Statement
Not applicable.
Informed Consent Statement
Not applicable.
Data Availability Statement
Not applicable.
Acknowledgments
We thank group members of Solgar Italia Multinutrient S.p.A. for their thorough review and helpful discussions during the preparation of this manuscript and for their help in elaborating the search strategy.
Conflicts of Interest
The authors declare no conflict of interest.
References
- Frackowiak, R.S. Human Brain Function; Elsevier: Amsterdam, The Netherlands, 2004. [Google Scholar]
- Gómez-Pinilla, F. Brain foods: The effects of nutrients on brain function. Nat. Rev. Neurosci. 2008, 9, 568–578. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Williams, R.J.; Mohanakumar, K.P.; Beart, P.M. Neuro-Nutraceuticals: The Path to Brain Health via Nourishment Is Not So Distant; Elsevier: Amsterdam, The Netherlands, 2015. [Google Scholar]
- Cian, R.E.; Drago, S.R.; De Medina, F.S.; Martínez-Augustin, O. Proteins and carbohydrates from red seaweeds: Evidence for beneficial effects on gut function and microbiota. Mar. Drugs 2015, 13, 5358–5383. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Reilly, P.; O’doherty, J.; Pierce, K.; Callan, J.; O’sullivan, J.; Sweeney, T. The effects of seaweed extract inclusion on gut morphology, selected intestinal microbiota, nutrient digestibility, volatile fatty acid concentrations and the immune status of the weaned pig. Animal 2008, 2, 1465–1473. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Strandwitz, P. Neurotransmitter modulation by the gut microbiota. Brain Res. 2018, 1693, 128–133. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cornish, M.L.; Critchley, A.T.; Mouritsen, O.G. Consumption of seaweeds and the human brain. J. Appl. Phycol. 2017, 29, 2377–2398. [Google Scholar] [CrossRef] [Scilit]
- Rosa, G.P.; Tavares, W.R.; Sousa, P.; Seca, A.M.; Pinto, D.C. Seaweed secondary metabolites with beneficial health effects: An overview of successes in in vivo studies and clinical trials. Mar. Drugs 2020, 18, 8. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pereira, L.; Valado, A. The Seaweed Diet in Prevention and Treatment of the Neurodegenerative Diseases. Mar. Drugs 2021, 19, 128. [Google Scholar] [CrossRef] [Scilit]
- Wang, Y.; Chang, C.-F.; Chou, J.; Chen, H.-L.; Deng, X.; Harvey, B.K.; Cadet, J.L.; Bickford, P.C. Dietary supplementation with blueberries, spinach, or spirulina reduces ischemic brain damage. Exp. Neurol. 2005, 193, 75–84. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Miranda, M.; Cintra, R.; Barros, S.d.M.; Mancini-Filho, J. Antioxidant activity of the microalga Spirulina maxima. Braz. J. Med. Biol. Res. 1998, 31, 1075–1079. [Google Scholar] [CrossRef] [Scilit]
- Kim, J.H.; Lee, N.S.; Jeong, Y.G.; Lee, J.-H.; Kim, E.J.; Han, S.Y. Protective efficacy of an Ecklonia cava extract used to treat transient focal ischemia of the rat brain. Anat. Cell Biol. 2012, 45, 103. [Google Scholar] [CrossRef] [Scilit]
- Um, M.Y.; Lim, D.W.; Son, H.J.; Cho, S.; Lee, C. Phlorotannin-rich fraction from Ishige foliacea brown seaweed prevents the scopolamine-induced memory impairment via regulation of ERK-CREB-BDNF pathway. J. Funct. Foods 2018, 40, 110–116. [Google Scholar] [CrossRef] [Scilit]
- Allaert, F.-A.; Demais, H.; Collén, P.N. A randomized controlled double-blind clinical trial comparing versus placebo the effect of an edible algal extract (Ulva Lactuca) on the component of depression in healthy volunteers with anhedonia. BMC Psychiatry 2018, 18, 215. [Google Scholar] [CrossRef] [Scilit]
- Reid, S.N.; Ryu, J.-K.; Kim, Y.; Jeon, B.H. The effects of fermented Laminaria japonica on short-term working memory and physical fitness in the elderly. Evid. Based Complementary Altern. Med. 2018, 2018, 8109621. [Google Scholar]
- Haskell-Ramsay, C.F.; Jackson, P.A.; Dodd, F.L.; Forster, J.S.; Bérubé, J.; Levinton, C.; Kennedy, D.O. Acute post-prandial cognitive effects of brown seaweed extract in humans. Nutrients 2018, 10, 85. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hannan, M.; Dash, R.; Haque, M.; Mohibbullah, M.; Sohag, A.A.M.; Rahman, M.; Uddin, M.J.; Alam, M.; Moon, I.S. Neuroprotective potentials of marine algae and their bioactive metabolites: Pharmacological insights and therapeutic advances. Mar. Drugs 2020, 18, 347. [Google Scholar] [CrossRef] [Scilit]
- Khan, Z.; Bhadouria, P.; Bisen, P. Nutritional and therapeutic potential of Spirulina. Curr. Pharm. Biotechnol. 2005, 6, 373–379. [Google Scholar] [CrossRef] [Scilit]
- Clément, G.; Giddey, C.; Menzi, R. Amino acid composition and nutritive value of the alga Spirulina maxima. J. Sci. Food Agric. 1967, 18, 497–501. [Google Scholar] [CrossRef] [Scilit]
- Tomaselli, L. Morphology, ultrastructure and taxonomy of Arthrospira (Spirulina) maxima and Arthrospira (Spirulina) platensis. In Spirulina Platensis (Arthrospira): Physiology, Cell-Biology and Biotechnology; Taylor & Francis: Abingdon, UK, 1997; pp. 1–16. [Google Scholar]
- Belay, A. Spirulina (Arthrospira): Production and quality assurance. In Spirulina in Human Nutrition and Health; CRC Press: Boca Raton, FL, USA, 2008; Volume 1. [Google Scholar]
- Babadzhanov, A.; Abdusamatova, N.; Yusupova, F.; Faizullaeva, N.; Mezhlumyan, L.; Malikova, M.K. Chemical Composition of Spirulina platensis Cultivated in Uzbekistan. Chem. Nat. Compd. 2004, 40, 276–279. [Google Scholar] [CrossRef] [Scilit]
- Vonshak, A. Spirulina Platensis Arthrospira: Physiology, Cell-Biology and Biotechnology; CRC Press: Boca Raton, FL, USA, 1997. [Google Scholar]
- Liestianty, D.; Rodianawati, I.; Arfah, R.A.; Assa, A. Nutritional analysis of spirulina sp to promote as superfood candidate. IOP Conf. Ser. Mater. Sci. Eng. 2019, 509, 012031. [Google Scholar] [CrossRef] [Scilit]
- Karkos, P.; Leong, S.; Karkos, C.; Sivaji, N.; Assimakopoulos, D. Spirulina in clinical practice: Evidence-based human applications. Evid. Based Complementary Altern. Med. 2011, 2011, 531053. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kennedy, D.O. B vitamins and the brain: Mechanisms, dose and efficacy—A review. Nutrients 2016, 8, 68. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wells, M.L.; Potin, P.; Craigie, J.S.; Raven, J.A.; Merchant, S.S.; Helliwell, K.E.; Smith, A.G.; Camire, M.E.; Brawley, S.H. Algae as nutritional and functional food sources: Revisiting our understanding. J. Appl. Phycol. 2017, 29, 949–982. [Google Scholar] [CrossRef] [Scilit]
- Makkar, R.; Behl, T.; Bungau, S.; Zengin, G.; Mehta, V.; Kumar, A.; Uddin, M.; Ashraf, G.M.; Abdel-Daim, M.M.; Arora, S. Nutraceuticals in neurological disorders. Int. J. Mol. Sci. 2020, 21, 4424. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sorrenti, V.; Fortinguerra, S.; Caudullo, G.; Buriani, A. Deciphering the Role of Polyphenols in Sports Performance: From Nutritional Genomics to the Gut Microbiota toward Phytonutritional Epigenomics. Nutrients 2020, 12, 1265. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sorrenti, V.; Ali, S.; Mancin, L.; Davinelli, S.; Paoli, A.; Scapagnini, G. Cocoa Polyphenols and Gut Microbiota Interplay: Bioavailability, Prebiotic Effect, and Impact on Human Health. Nutrients 2020, 12, 1908. [Google Scholar] [CrossRef] [Scilit]
- Neyrinck, A.M.; Taminiau, B.; Walgrave, H.; Daube, G.; Cani, P.D.; Bindels, L.B.; Delzenne, N.M. Spirulina protects against hepatic inflammation in aging: An effect related to the modulation of the gut microbiota? Nutrients 2017, 9, 633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hu, J.; Li, Y.; Pakpour, S.; Wang, S.; Pan, Z.; Liu, J.; Wei, Q.; She, J.; Cang, H.; Zhang, R.X. Dose effects of orally administered Spirulina suspension on colonic microbiota in healthy mice. Front. Cell. Infect. Microbiol. 2019, 9, 243. [Google Scholar] [CrossRef] [Scilit]
- Morais, L.H.; Schreiber, H.L.; Mazmanian, S.K. The gut microbiota–brain axis in behaviour and brain disorders. Nat. Rev. Microbiol. 2021, 119, 241–255. [Google Scholar] [CrossRef] [Scilit]
- Westfall, S.; Lomis, N.; Kahouli, I.; Dia, S.Y.; Singh, S.P.; Prakash, S. Microbiome, probiotics and neurodegenerative diseases: Deciphering the gut brain axis. Cell. Mol. Life Sci. 2017, 74, 3769–3787. [Google Scholar] [CrossRef] [Scilit]
- Yu, T.; Wang, Y.; Chen, X.; Xiong, W.; Tang, Y.; Lin, L. Spirulina platensis alleviates chronic inflammation with modulation of gut microbiota and intestinal permeability in rats fed a high-fat diet. J. Cell. Mol. Med. 2020, 24, 8603–8613. [Google Scholar] [CrossRef] [Scilit]
- Xie, Y.; Li, W.; Zhu, L.; Zhai, S.; Qin, S.; Du, Z. Effects of phycocyanin in modulating the intestinal microbiota of mice. MicrobiologyOpen 2019, 8, e00825. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Park, J.-C.; Han, S.-H.; Byun, M.S.; Yi, D.; Lee, J.H.; Park, K.; Lee, D.Y.; Mook-Jung, I. Low serum phosphorus correlates with cerebral Aβ deposition in cognitively impaired subjects: Results from the KBASE study. Front. Aging Neurosci. 2017, 9, 362. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Slutsky, I.; Abumaria, N.; Wu, L.-J.; Huang, C.; Zhang, L.; Li, B.; Zhao, X.; Govindarajan, A.; Zhao, M.-G.; Zhuo, M. Enhancement of learning and memory by elevating brain magnesium. Neuron 2010, 65, 165–177. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Takeda, A. Manganese action in brain function. Brain Res. Rev. 2003, 41, 79–87. [Google Scholar] [CrossRef] [Scilit]
- Sperringer, J.E.; Addington, A.; Hutson, S.M. Branched-chain amino acids and brain metabolism. Neurochem. Res. 2017, 42, 1697–1709. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fernstrom, J.D. Dietary amino acids and brain function. J. Am. Diet. Assoc. 1994, 94, 71–77. [Google Scholar] [CrossRef] [Scilit]
- Kapoor, R.; Huang, Y.-S. Gamma linolenic acid: An antiinflammatory omega-6 fatty acid. Curr. Pharm. Biotechnol. 2006, 7, 531–534. [Google Scholar] [CrossRef] [Scilit]
- Biessels, G.J.; Smale, S.; Duis, S.E.; Kamal, A.; Gispen, W.H. The effect of gamma-linolenic acid–alpha-lipoic acid on functional deficits in the peripheral and central nervous system of streptozotocin-diabetic rats. J. Neurol. Sci. 2001, 182, 99–106. [Google Scholar] [CrossRef] [Scilit]
- Desai, K.; Sivakami, S. Purification and biochemical characterization of a superoxide dismutase from the soluble fraction of the cyanobacterium, Spirulina platensis. World J. Microbiol. Biotechnol. 2007, 23, 1661–1666. [Google Scholar] [CrossRef] [Scilit]
- Bachstetter, A.D.; Jernberg, J.; Schlunk, A.; Vila, J.L.; Hudson, C.; Cole, M.J.; Shytle, R.D.; Tan, J.; Sanberg, P.R.; Sanberg, C.D. Spirulina promotes stem cell genesis and protects against LPS induced declines in neural stem cell proliferation. PLoS ONE 2010, 5, e10496. [Google Scholar] [CrossRef] [Scilit]
- Patil, J.; Matte, A.; Nissbrandt, H.; Mallard, C.; Sandberg, M. Sustained effects of neonatal systemic lipopolysaccharide on IL-1β and Nrf2 in adult rat substantia nigra are partly normalized by a spirulina-enriched diet. Neuroimmunomodulation 2016, 23, 250–259. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Patil, J.; Matte, A.; Mallard, C.; Sandberg, M. Spirulina diet to lactating mothers protects the antioxidant system and reduces inflammation in post-natal brain after systemic inflammation. Nutr. Neurosci. 2018, 21, 59–69. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Fried, R. Superoxide dismutase activity in the nervous system. J. Neurosci. Res. 1979, 4, 435–441. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hwang, J.-H.; Lee, I.-T.; Jeng, K.-C.; Wang, M.-F.; Hou, R.C.-W.; Wu, S.-M.; Chan, Y.-C. Spirulina prevents memory dysfunction, reduces oxidative stress damage and augments antioxidant activity in senescence-accelerated mice. J. Nutr. Sci. Vitaminol. 2011, 57, 186–191. [Google Scholar] [CrossRef] [Scilit]
- Koh, E.-J.; Kim, K.-J.; Song, J.-H.; Choi, J.; Lee, H.Y.; Kang, D.-H.; Heo, H.J.; Lee, B.-Y. Spirulina maxima extract ameliorates learning and memory impairments via inhibiting GSK-3β phosphorylation induced by intracerebroventricular injection of amyloid-β 1–42 in mice. Int. J. Mol. Sci. 2017, 18, 2401. [Google Scholar] [CrossRef] [Scilit]
- Pabon, M.M.; Jernberg, J.N.; Morganti, J.; Contreras, J.; Hudson, C.E.; Klein, R.L.; Bickford, P.C. A Spirulina-Enhanced diet provides neuroprotection in an α-synuclein model of Parkinson’s disease. PLoS ONE 2012, 7, e45256. [Google Scholar] [CrossRef] [Scilit]
- Lima, F.A.V.; Joventino, I.P.; Joventino, F.P.; de Almeida, A.C.; Neves, K.R.T.; do Carmo, M.R.; Leal, L.K.A.M.; de Andrade, G.M.; de Barros Viana, G.S. Neuroprotective activities of Spirulina platensis in the 6-OHDA model of Parkinson’s disease are related to its anti-inflammatory effects. Neurochem. Res. 2017, 42, 3390–3400. [Google Scholar] [CrossRef] [Scilit]
- Choi, W.Y.; Kang, D.H.; Lee, H.Y. Effect of fermented Spirulina maxima extract on cognitive-enhancing activities in mice with scopolamine-induced dementia. Evid. Based Complementary Altern. Med. 2018, 2018, 7218504. [Google Scholar] [CrossRef] [Scilit]
- Chan, Y.-C.; Hwang, J.-H. Effects of Spirulina on the functions and redox status of auditory system in senescence-accelerated prone-8 mice. PLoS ONE 2017, 12, e0178916. [Google Scholar] [CrossRef] [Scilit]
- Gargouri, M.; Ghorbel-Koubaa, F.; Bonenfant-Magné, M.; Magné, C.; Dauvergne, X.; Ksouri, R.; Krichen, Y.; Abdelly, C.; El Feki, A. Spirulina or dandelion-enriched diet of mothers alleviates lead-induced damages in brain and cerebellum of newborn rats. Food Chem. Toxicol. 2012, 50, 2303–2310. [Google Scholar] [CrossRef] [Scilit]
- Galal, M.K.; Elleithy, E.M.; Abdrabou, M.I.; Yasin, N.A.; Shaheen, Y.M. Modulation of caspase-3 gene expression and protective effects of garlic and spirulina against CNS neurotoxicity induced by lead exposure in male rats. NeuroToxicology 2019, 72, 15–28. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Banji, D.; Banji, O.J.; Pratusha, N.G.; Annamalai, A. Investigation on the role of Spirulina platensis in ameliorating behavioural changes, thyroid dysfunction and oxidative stress in offspring of pregnant rats exposed to fluoride. Food Chem. 2013, 140, 321–331. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ibrahim, F.; Nomier, M.A.; Sabik, L.M.; Shaheen, M.A. Manganese-induced neurotoxicity and the potential protective effects of lipoic acid and Spirulina platensis. Toxicol. Mech. Methods 2020, 30, 497–507. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Thaakur, S.; Sravanthi, R. Neuroprotective effect of Spirulina in cerebral ischemia–reperfusion injury in rats. J. Neural Transm. 2010, 117, 1083–1091. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Madhavadas, S.; Subramanian, S. Combination of Spirulina with glycyrrhizin prevents cognitive dysfunction in aged obese rats. Indian J. Pharmacol. 2015, 47, 39. [Google Scholar]
- Zhu, H.-Z.; Zhang, Y.; Zhu, M.-J.; Wu, R.-L.; Zeng, Z.-G. Protective effects of spirulina on hippocampal injury in exercise-fatigue mice and its mechanism. Chin. J. Appl. Physiol. 2018, 34, 562. [Google Scholar]
- Okamoto, T.; Kawashima, H.; Osada, H.; Toda, E.; Homma, K.; Nagai, N.; Imai, Y.; Tsubota, K.; Ozawa, Y. Dietary spirulina supplementation protects visual function from photostress by suppressing retinal neurodegeneration in mice. Transl. Vis. Sci. Technol. 2019, 8, 20. [Google Scholar] [CrossRef] [Scilit]
- Zhao, B.; Cui, Y.; Fan, X.; Qi, P.; Liu, C.; Zhou, X.; Zhang, X. Anti-obesity effects of Spirulina platensis protein hydrolysate by modulating brain-liver axis in high-fat diet fed mice. PLoS ONE 2019, 14, e0218543. [Google Scholar] [CrossRef] [Scilit]
- Moradi-Kor, N.; Ghanbari, A.; Rashidipour, H.; Bandegi, A.R.; Yousefi, B.; Barati, M.; Kokhaei, P.; Rashidy-Pour, A. Therapeutic effects of spirulina platensis against adolescent stress-induced oxidative stress, brain-derived neurotrophic factor alterations and morphological remodeling in the amygdala of adult female rats. J. Exp. Pharmacol. 2020, 12, 75. [Google Scholar] [CrossRef] [Scilit]
- Sinha, S.; Patro, N.; Tiwari, P.; Patro, I.K. Maternal Spirulina supplementation during pregnancy and lactation partially prevents oxidative stress, glial activation and neuronal damage in protein malnourished F1 progeny. Neurochem. Int. 2020, 141, 104877. [Google Scholar] [CrossRef] [Scilit]
- Khalil, S.R.; Khalifa, H.A.; Abdel-Motal, S.M.; Mohammed, H.H.; Elewa, Y.H.; Mahmoud, H.A. Spirulina platensis attenuates the associated neurobehavioral and inflammatory response impairments in rats exposed to lead acetate. Ecotoxicol. Environ. Saf. 2018, 157, 255–265. [Google Scholar] [CrossRef] [Scilit]
- Park, H.J.; Lee, Y.J.; Ryu, H.K.; Kim, M.H.; Chung, H.W.; Kim, W.Y. A randomized double-blind, placebo-controlled study to establish the effects of spirulina in elderly Koreans. Ann. Nutr. Metab. 2008, 52, 322–328. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Johnson, M.; Hassinger, L.; Davis, J.; Devor, S.T.; DiSilvestro, R.A. A randomized, double blind, placebo controlled study of spirulina supplementation on indices of mental and physical fatigue in men. Int. J. Food Sci. Nutr. 2016, 67, 203–206. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Hernández-Lepe, M.A.; Wall-Medrano, A.; López-Díaz, J.A.; Juárez-Oropeza, M.A.; Luqueño-Bocardo, O.I.; Hernández-Torres, R.P.; Ramos-Jiménez, A. Hypolipidemic effect of Arthrospira (Spirulina) maxima supplementation and a systematic physical exercise program in overweight and obese men: A double-blind, randomized, and crossover controlled trial. Mar. Drugs 2019, 17, 270. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Masuda, K.; Chitundu, M. Multiple micronutrient supplementation using Spirulina platensis during the first 1000 days is positively associated with development in children under five years: A follow up of a randomized trial in Zambia. Nutrients 2019, 11, 730. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Miczke, A.; Szulinska, M.; Hansdorfer-Korzon, R.; Kregielska-Narozna, M.; Suliburska, J.; Walkowiak, J.; Bogdanski, P. Effects of spirulina consumption on body weight, blood pressure, and endothelial function in overweight hypertensive Caucasians: A double-blind, placebo-controlled, randomized trial. Eur. Rev. Med. Pharm. Sci. 2016, 20, 150–156. [Google Scholar]
- Zeinalian, R.; Farhangi, M.A.; Shariat, A.; Saghafi-Asl, M. The effects of Spirulina Platensis on anthropometric indices, appetite, lipid profile and serum vascular endothelial growth factor (VEGF) in obese individuals: A randomized double blinded placebo controlled trial. BMC Complementary Altern. Med. 2017, 17, 225. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Martínez-Sámano, J.; Torres-Montes de Oca, A.; Luqueño-Bocardo, O.I.; Torres-Durán, P.V.; Juárez-Oropeza, M.A. Spirulina maxima decreases endothelial damage and oxidative stress indicators in patients with systemic arterial hypertension: Results from exploratory controlled clinical trial. Mar. Drugs 2018, 16, 496. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Buriani, A.; Fortinguerra, S.; Carrara, M.; Pelkonen, O. Systems network pharmaco-toxicology in the study of herbal medicines. In Toxicology of Herbal Products; Springer: Berlin/Heidelberg, Germany, 2017; pp. 129–164. [Google Scholar]
- Buriani, A.; Fortinguerra, S.; Sorrenti, V.; Caudullo, G.; Carrara, M. Essential Oil Phytocomplex Activity, a Review with a Focus on Multivariate Analysis for a Network Pharmacology-Informed Phytogenomic Approach. Molecules 2020, 25, 1833. [Google Scholar] [CrossRef] [Scilit] [PubMed]

Publisher’s Note: MDPI stays neutral with regard to jurisdictional claims in published maps and institutional affiliations. |
© 2021 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).