


Abstract
Astringent persimmons (Diospyros kaki Thunb.) require effective postharvest deastringency treatments due to their high soluble tannin content at harvest. While high CO2 and ethylene are commonly used to remove astringency, their different effects on fruit firmness and quality require cultivar-specific approaches. This study investigated the transcriptomic and biochemical responses of ‘Daebong’ persimmon to high CO2 and ethylene treatments during deastringency. Both treatments significantly decreased soluble tannin and total phenolic content, enhancing fruit edibility. However, the firmness was maintained under high levels of CO2, but it decreased quickly after exposure to ethylene. RNA-Seq analysis identified 2271 differentially expressed genes (DEGs) and revealed distinct transcriptional signatures for each treatment. CO2 treatment activated hypoxia-responsive genes, stress-related transcription factors (e.g., WRKY, ERF14/26), and components of antioxidant defense (e.g., GSTU17, peroxidases), which contributed to oxidative stress reduction and preservation of firmness. On the other hand, ethylene treatment increased ethylene biosynthesis (ACS), signaling (EIN3-binding F-box), and ripening-related genes (polygalacturonase, laccase, ERF061/113), which promote cell wall degradation and softening. Functional enrichment analysis revealed that various regulatory mechanisms are responsible for the insolubilization of tannins, loss of antioxidants, and changes in firmness. These findings provide new insights into the molecular responses of pollination-constant astringent (PCA) persimmons, particularly the ‘Daebong’ cultivar, to postharvest deastringency treatments for the development of more effective postharvest management strategies. The results suggest that high CO2 helps maintain fruit quality by promoting stress adaptation and suppressing pathways that lead to softening, whereas ethylene accelerates the ripening process by activating signaling pathways associated with ethylene.
1. Introduction
Persimmon (Diospyros kaki Thunb.) is a climacteric fruit widely cultivated in East Asia, particularly in China, Japan, and South Korea, which together account for more than 94.4% of global production [1]. Among the diverse astringent cultivars, ‘Daebong’, a traditional Korean cultivar classified as pollination-constant astringent (PCA), is highly valued for its rich flavor and is widely used for both fresh consumption and processing [2,3,4]. Unlike non-astringent cultivars, such as pollination-constant non-astringent (PCNA) types, PCA-type persimmons maintain high levels of soluble tannin at harvest. This results in a pronounced astringent taste that limits their direct edibility [5,6].
During the development of fruit, oriental persimmons accumulate water-soluble tannins in the tannin cells of their flesh, which are responsible for the characteristic astringent taste [5] These compounds interact with salivary proteins, resulting in an unpleasant drying or puckering sensation in the mouth [7]. Therefore, postharvest deastringency treatment is essential for the commercial handling and consumer acceptance of astringent cultivars like ‘Daebong’ [2]. Traditional treatments such as ethanol exposure [8], hot water immersion [9], and natural ripening have been reported to induce acetaldehyde accumulation, which polymerizes soluble tannins into insoluble forms [6]. However, these methods often lead to inconsistent quality and require extended treatment durations. Among the currently available methods, high CO2 and exogenous ethylene treatments are commonly used for their rapid and reliable deastringency effects [3,10]. High CO2 treatment creates anaerobic conditions, activating the pyruvate decarboxylase (PDC) and alcohol dehydrogenase (ADH) pathways, which leads to the accumulation of acetaldehyde [11,12,13]. In contrast, ethylene treatment enhances deastringency by regulating hormones and activating enzymes associated with ripening [14,15,16]. However, the two treatments have different effects on fruit firmness and postharvest handling. High CO2 treatment is generally effective in preserving flesh firmness and reducing astringency. In contrast, exposure to ethylene tends to cause rapid softening of the fruit by increasing the content of water-soluble pectin and promoting the degradation of cell walls [2,17,18].
Previous transcriptomic studies on deastringency have predominantly concentrated on Japanese PCNA cultivars [19] and Chinese PCA cultivars [20]. However, information regarding traditional Korean PCA-type cultivars, such as ‘Daebong’-a widely cultivated astringent persimmon in South Korea-remains relatively limited. Understanding the unique molecular and biochemical responses of ‘Daebong’ to high CO2 and ethylene is essential for optimizing postharvest treatments, given the commercial importance of firmness retention and consumer-preferred soft textures.
Therefore, this study aimed to investigate the specific transcriptomic and biochemical responses of the ‘Daebong’ persimmon cultivar to high CO2 and ethylene treatments. The research focused on identifying significant changes in gene expression, firmness characteristics, and shifts in antioxidant-related metabolites that occur during the deastringency process. The findings will contribute to the development of more effective postharvest management strategies for PCA-type persimmons.
2. Materials and Methods
2.1. Plant Materials, High CO2 and Ethylene Treatments
Mature ‘Daebong’ astringent persimmons (Diospyros kaki Thunb.) were harvested on 21 October 2023, from an orchard in Yeongam, Jeollanam-do, South Korea (latitude 34.84698° N, longitude 126.77564° E). Only fruits that were uniform in size and free from visible defects or external damage were selected for subsequent treatment. Immediately after harvest, the fruits were transported to the Postharvest Management Laboratory at the Department of Horticulture Science, Kangwon National University. At harvest, fruits of the ‘Daebong’ cultivar had an average fresh weight of 300 g, firmness of 21.31 N, and soluble tannin content of 5.52 g kg−1. For the deastringency treatments, 20 selected fruits were placed in 62 L airtight plastic chambers without any packaging to ensure uniform gas exposure. For the high CO2 treatment, 95% CO2 (purity ≥ 99.9%) was introduced into the chambers and maintained for 24 h at 25 °C, based on the total chamber volume (62 L) [21,22]. For the ethylene treatment, 100 μL L−1 ethylene (purity ≥ 99.9%) was applied under the same chamber and temperature conditions for 24 h [2,18]. Internal air circulation within the chambers was maintained using a small fan (EC12025L24S, Evercool Thermal Ltd., Dongguan, China) to ensure uniform gas distribution. Control fruits were held under identical chamber conditions (25 °C, 24 h) without high CO2 or ethylene treatments. Tissue samples were collected at three different time points: before the treatment began (0 days), after 1 day of high CO2 treatment, and after 4 days of ethylene treatment. These samples were used for transcriptome profiling, measuring pectin content, ethanol-insoluble solids (EIS), and polygalacturonase (PG) activity. The collected fruit flesh was immediately frozen in liquid nitrogen and stored at −80 °C until analysis. Simultaneously, fruit firmness, ethylene production, and respiration rates were measured using intact fruits. For the biochemical analyses of secondary metabolites and antioxidant activity, three biological replicates from each treatment group were also stored at −80 °C and subsequently freeze-dried using an FDT-8650 vacuum freeze dryer (Operon, Gimpo, Republic of Korea). The dried tissues were ground into a powder using a food grinder, filtered through a 40 μm mesh sieve, sealed in low-density polyethylene (LDPE) pouches, and preserved at −20 °C until extraction for analysis.
2.2. RNA Extraction
The overall transcriptome analysis followed the protocol described by [23]. Total RNA was extracted using the hybrid-RTM kit (Gene All Biotechnology Co., Seoul, Republic of Korea). RNA quality and quantity were assessed using the Agilent 2100 Bioanalyzer (Agilent Technologies Inc., Santa Clara, CA, USA). Only RNA samples with concentrations ranging from 1 to 10 µg and an RNA Integrity Number (RIN) above 8.0 were selected for downstream applications. Equal amounts of high-quality total RNA from each sampling time point were pooled to construct three RNA-Seq libraries corresponding to the untreated control, high CO2, and ethylene treatment groups.
2.3. cDNA Library Construction, Sequencing, and Quality Control
cDNA libraries were prepared using the TruSeq RNA Sample Preparation Kit v2 (Illumina Inc., San Diego, CA, USA) according to the manufacturer’s instructions. Paired-end sequencing was performed on an Illumina NovaSeq 6000 platform at Macrogen Inc. (Seoul, Republic of Korea). Raw reads were processed using Trimmomatic v0.39 (http://www.usadellab.org/cms/?page=trimmomatic (accessed on 4 December 2023)) with the following parameters: removal of adapter sequences, trimming of low-quality bases with Phred scores below 20, and exclusion of reads shorter than 50 bp. Raw reads were processed using Trimmomatic v0.39 (http://www.usadellab.org/cms/?page=trimmomatic (accessed on 4 December 2023)) with the following parameters: removal of adapter sequences, trimming of low-quality bases with Phred scores below 20, and exclusion of reads shorter than 50 bp [24].
2.4. De Novo Assembly and Contig Filtering
Sequencing reads were de novo assembled into contigs using the Trinity v2.13.2 with default parameters (https://github.com/trinityrnaseq/trinityrnaseq/wiki (accessed on 4 December 2023)). Redundant contigs were removed using CD-HIT-EST v4.8.1 with a sequence identity threshold of 0.9, retaining only the longest sequence among highly similar contigs (https://github.com/weizhongli/cdhit/releases (accessed on 4 December 2023)). The quality of the assembled transcriptome was evaluated by mapping clean reads back to the contigs using BWA v0.7.17 (https://github.com/lh3/bwa (accessed on 4 December 2023)) and SamTools v1.13 (https://www.htslib.org (accessed on 4 December 2023)). Contigs with fewer than five mapped reads were excluded from downstream analyses [25].
2.5. Identification of DEGs and Functional Enrichment Analysis
To identify coding sequences within the contigs, TransDecoder v5.5.0 (https://github.com/TransDecoder/TransDecoder/wiki (accessed on 4 December 2023)) was used. The TransDecoder.LongOrfs module was applied to predict the longest open reading frames (ORFs), which were then annotated by homology searches against the UniProt database using DIAMOND v2.1.8.162 and the Pfam database using HMMER v3.3 (http://hmmer.org/ (accessed on 4 December 2023)). The final coding sequence set was defined using the TransDecoder.Predict module. Redundant sequences were filtered using CD-HIT v4.8.1 at 95% identity, based on predicted protein sequences.
For expression analysis, clean reads were aligned to the assembled contigs using BWA v0.7.17, and read counts were generated using Samtools v1.13. Differentially expressed genes (DEGs) were identified using DESeq2 v1.36.0 with an adjusted p-value (FDR) < 0.05 and |log2 fold change| > 2 as thresholds to determine significant expression changes among the three treatment groups.
Functional annotation of the predicted proteins was conducted using DIAMOND v2.1.8.162 against the NCBI non-redundant (nr) database. InterProScan v5.62-94.0 (https://www.ebi.ac.uk/interpro/search/sequence/ (accessed on 4 December 2023)) was also employed to identify conserved protein domains. All annotation results were integrated using BLAST2GO (https://www.blast2go.com/ (accessed on 4 December 2023) to assign Gene Ontology (GO) terms and to perform enrichment analysis. Transcriptome completeness was evaluated using BUSCO v5.3.2 with the eukaryota lineage dataset, providing a standardized measure of assembly quality based on the detection of conserved single-copy orthologs.
2.6. Firmness, Ethanol Insoluble (EIS), Pectin Content, and Polygalacturonase (PG) Activity
Fruit firmness was measured using a hardness meter (Rheometer, Sun Scientific Co., Ltd., Tokyo, Japan) fitted with a cylindrical stainless-steel probe, measuring 3 mm in diameter and having a flat end. Measurements were taken at the equatorial region of 15 randomly selected fruits, with two replicates per fruit. A maximum compression force of 98.1 N (equivalent to 10 kgf) was applied. The firmness values were recorded as the peak force required penetrating the surface of the fruit, following the methodology described by Baek et al. [2]. Ethanol-insoluble solids (EIS), total pectin content, and polygalacturonase (PG) activity were measured using established protocols with slight modifications, as described by Choi et al. [26] and Seo et al. [27]. EIS was extracted by homogenizing the fruit tissue in ethanol and recovering the insoluble fraction through centrifugation. Total pectin content was quantified using colorimetric analysis following acid extraction, while PG activity was evaluated by measuring the rate of hydrolysis of polygalacturonic acid under specific pH and temperature conditions.
2.7. Ethylene Production and Respiration Rate
The ethylene production and respiration rates of persimmon fruits were determined following the procedure described by Choi et al. [26], with slight modifications to the gas chromatography conditions according to the actual instrument settings. Intact fruits were sealed in 4 L airtight containers and incubated for 3 h at an ambient temperature. A 1 mL headspace gas sample was withdrawn from each container using a gas-tight syringe and injected into a gas chromatograph (Nexis GC-2030, Shimadzu Corporation, Kyoto, Japan) equipped with a BP20 fused silica capillary column (30 m × 0.25 mm i.d., 0.25 μm film thickness; SGE Analytical Science, Victoria, Australia) and a flame ionization detector (FID). The injector (SPL) and detector (FID) temperatures were both maintained at 250 °C. The column oven was set to 160 °C under isothermal conditions. Helium was used as the carrier gas at a constant total flow rate of 15.0 mL min−1 with a split ratio of 5.0. The make-up gas (He) flow was maintained at 24.0 mL min−1, while hydrogen and air flows for the FID were set to 32.0 mL min−1 and 200.0 mL min−1, respectively. The column pressure was maintained at approximately 195.7 kPa. The linear velocity was 46.6 cm s−1 and the purge flow was 3.0 mL min−1. The rate of ethylene production was expressed as microliters of C2H4 per kilogram of fruit per hour (μL C2H4 kg−1 h−1).
For respiration analysis, CO2 accumulation in the headspace was quantified using a headspace gas analyzer (GS 6600, Illinois Instruments, Inc., Johnsburg, IL, USA). CO2 concentration was measured at the beginning and after 3 h of incubation, and the respiration rate was calculated based on the increase in CO2 concentration over time. Results were expressed as milliliters of CO2 per kilogram per hour (mL CO2 kg−1 h−1).
2.8. Soluble Tannin Content and Total Phenolics
Soluble tannin was extracted from freeze-dried persimmon powder using 80% aqueous methanol by applying two sequential extraction steps: ultrasonication and orbital shaking (SI-600R, Medline Scientific, Oxfordshire, UK), each for 1 h at room temperature, followed the method described by Tewari et al. [28] (2017). The resulting extracts were centrifuged at 12,578× g for 15 min at 22 °C using a Mega-17R refrigerated centrifuge (Hanil Science Industrial, Gimpo, Republic of Korea). The supernatant was filtered through a 0.22 μm PTFE syringe filter and transferred into HPLC vials for chromatographic analysis.
Chromatographic separation was conducted using a high-performance liquid chromatography system (Nanospace SI-2, Shiseido Co., Kyoto, Japan) equipped with a photodiode array detector (PDA). A reversed-phase Cadenza 5CD-C18 column (4.6 × 250 mm, 5 μm; Imtakt Co., Kyoto, Japan) was employed, and column temperature was maintained at 40 °C. The detection wavelength was set at 270 nm. The mobile phase consisted of 0.1% (v/v) trifluoroacetic acid in distilled water (solvent A) and methanol (solvent B). The elution profile was programmed as follows: 0–5 min, 95:5 (A:B); 5–15 min, isocratic at 90:10; 15–30 min, linear gradient to 80:20; 30–45 min, isocratic at 80:20; followed by re-equilibration to initial conditions. The flow rate was set at 1.0 mL min−1, and the injection volume was 5 μL. All solvents were filtered through a 0.45 μm membrane filter and degassed before use. Tannic acid (Sigma-Aldrich, St. Louis, MO, USA) was used for calibration and quantification, and results were expressed in terms of tannic acid equivalents.
Total phenolic content was determined based on the modified Folin–Ciocalteu method, previously validated in our laboratory [29]. Briefly, 1 mL of ethanolic extract (equivalent to 1 mg of dry sample) or standard gallic acid solution was mixed with 1 mL of 10% Folin–Ciocalteu reagent, followed by the addition of 1 mL of 2% (w/v) sodium carbonate. The mixture was incubated in the dark for 90 min at room temperature. Absorbance was measured at 750 nm using a Spectramax i3 microplate reader (Molecular Devices, Sunnyvale, CA, USA). The concentration of phenolic compounds was calculated from a standard curve constructed with gallic acid, and the results were expressed as mg of gallic acid equivalents (GAE) per 100 g of dry sample (mg GAE 100 g−1).
2.9. Antioxidant Activities
For antioxidant analysis, finely powdered freeze-dried persimmon samples were extracted according to the protocol established by Baek et al. [29]. The antioxidant properties, including DPPH radical scavenging activity, Trolox-equivalent antioxidant capacity (ABTS), and ferric reducing antioxidant power (FRAP), were determined in triplicate. In addition, the reducing power assay was performed in triplicate following the method reported by Choi et al. [30].
2.10. Color Changes and Overall Sensory Evaluation
External fruit color parameters, including lightness (L*), redness (a*), yellowness (b*), and hue angle (h°), were measured on 15 fruits, with three measurements per fruit using a CR-400 Chroma Meter (Minolta, Tokyo, Japan). The total color difference (ΔE) before and after deastringency treatment was calculated as follows [31].
where ΔL*, Δa* and Δb* represent the mean changes in each color parameter.
Overall sensory evaluation, including deastringency, flavor, color, sweetness, and texture, were assessed by a panel of 10 trained graduate students using a five-point scale ranging from 1 (poor) to 5 (excellent), as described by Choi et al. [32].
2.11. Statistical Analysis of Quality Parameters
Statistical analysis of quality parameters was conducted as follows. All data were expressed as means ± standard errors, and significant differences among treatments were determined by analysis of variance (ANOVA) using SAS statistical software (SAS/STAT® 9.4; SAS Institute Inc., Cary, NC, USA) at a significance level of p < 0.05. When ANOVA indicated significance, Duncan’s multiple range test was applied for post hoc comparisons. For multivariate analysis, Pearson’s correlation analysis was performed to evaluate associations among the measured parameters. Prior to heatmap generation, VIP score calculation, and partial least squares discriminant analysis (PLS-DA), the dataset was normalized by median centering followed by autoscaling. Heatmaps visualization, VIP scores, and PLS-DA were performed using MetaboAnalyst 6.0 (https://www.metaboanalyst.ca/ (accessed on 11 August 2024)).
3. Results and Discussion
3.1. Assembly, Annotation, and DEGs
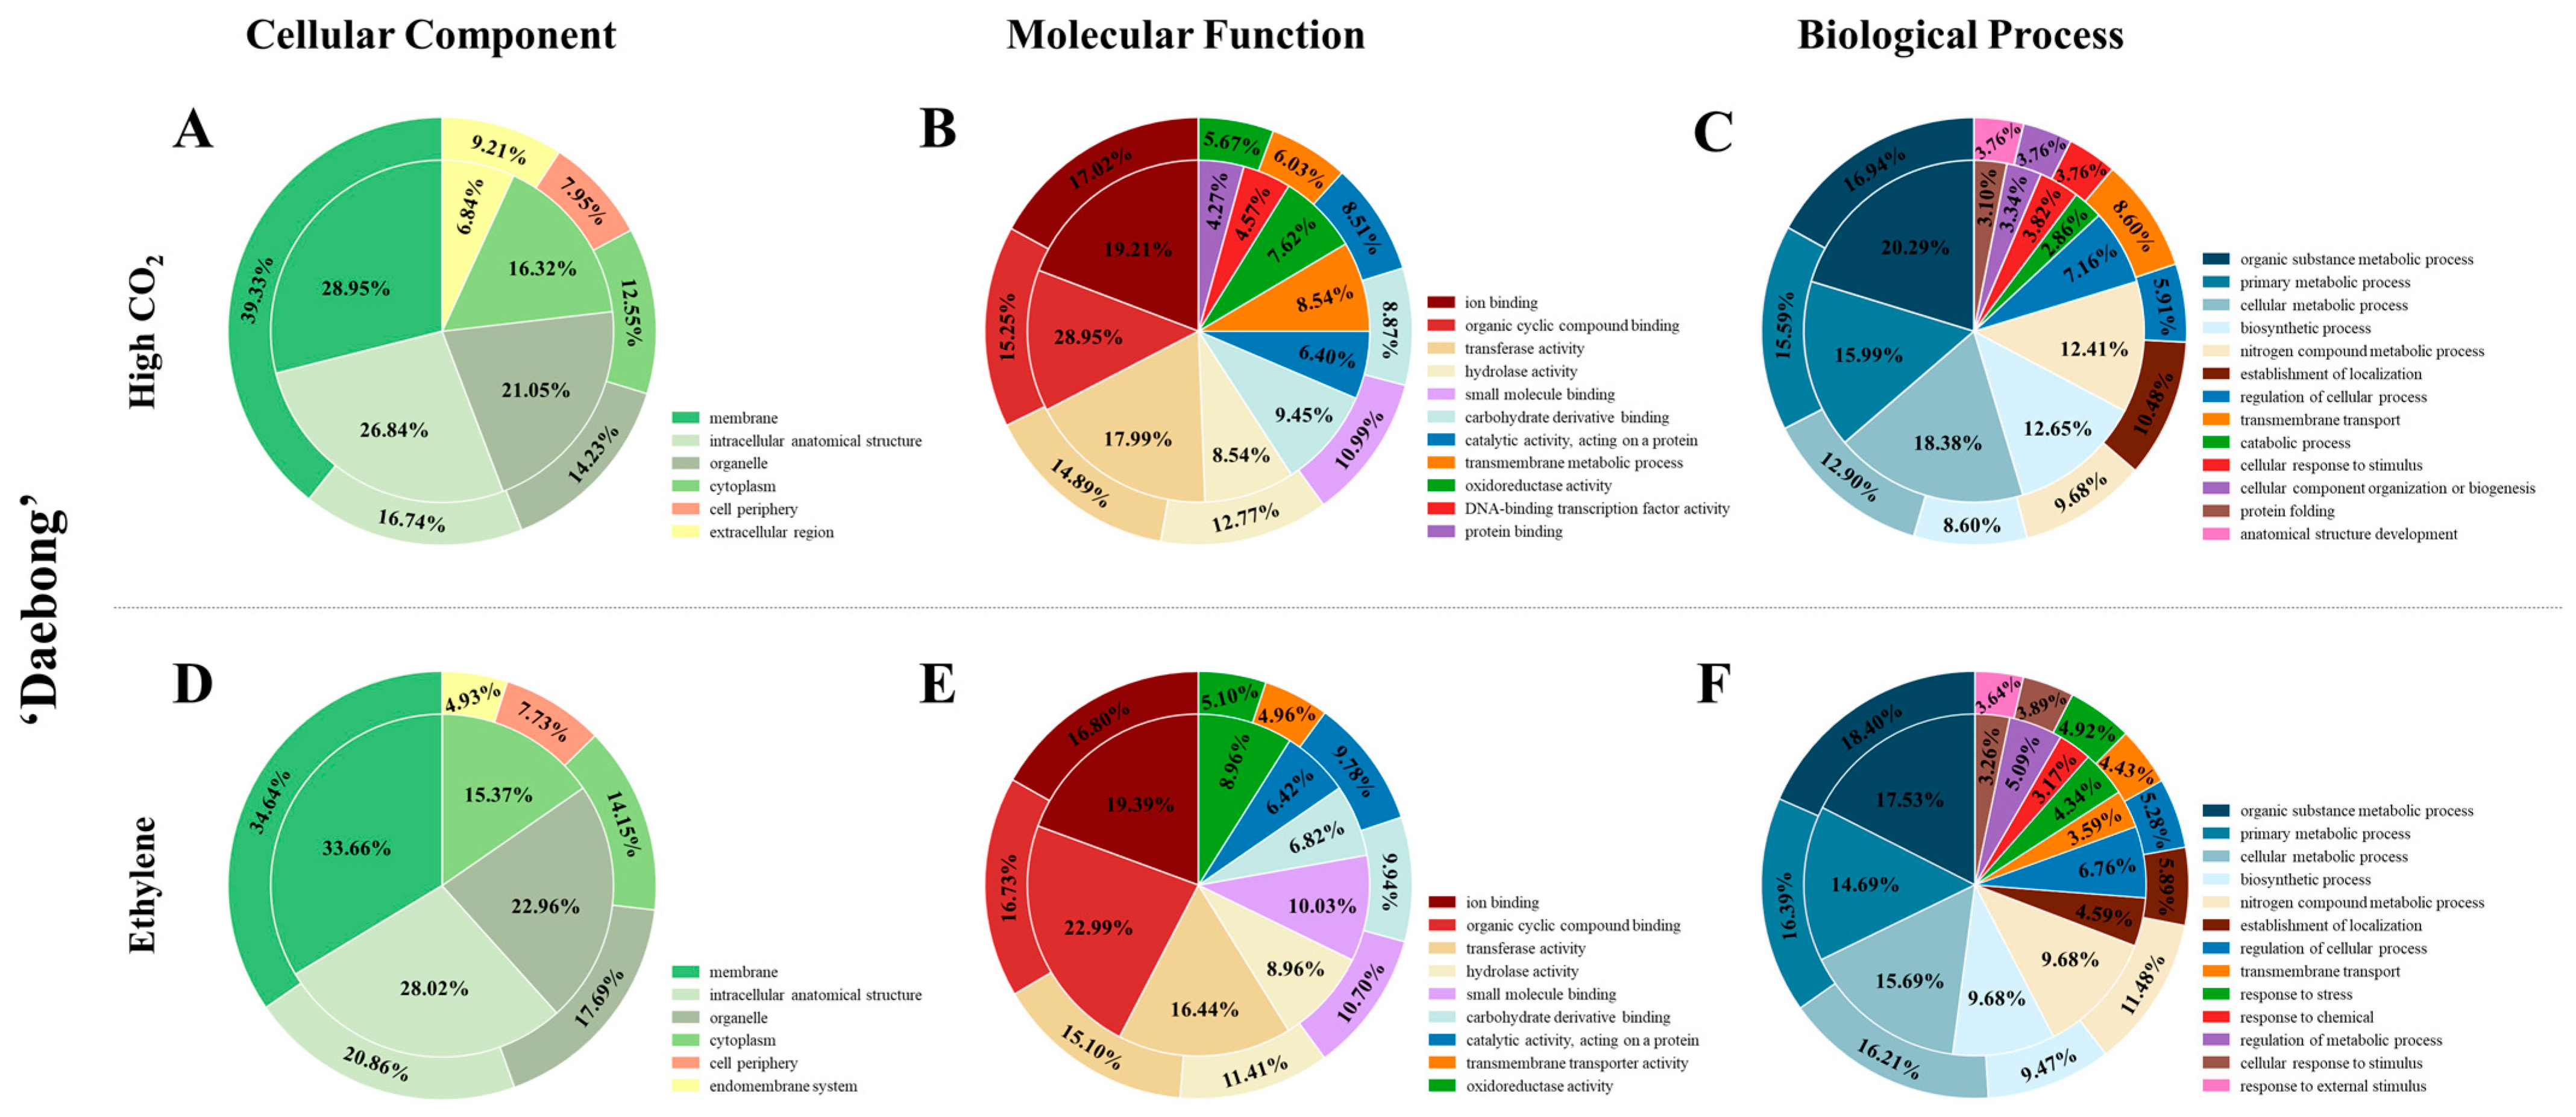
The summaries of raw, trimmed, and mapped data at harvest (control), and on the 1st and 4th days following deastringency treatments with high CO2 and ethylene at 25 °C are presented in Table 1. In this study, three ‘Daebong’ persimmon fruit transcriptome datasets were generated. The datasets were fruit at commercial harvest (control) and fruit at ‘ready to eat’ stage (high CO2-treated fruit on the 1st day and ethylene-treated fruit on the 4th day). The control, high CO2 and ethylene libraries produced an average of 67.20, 76.17 and 75.79 million reads, respectively, with corresponding mapped averages of 43.60, 44.37 and 47.46 million reads (Table 1) using a de novo approach. A total of 30,183 unigenes were identified with an average length of 1698 bp in the assembled sequences generated from RNA-Seq data. Table 1 also shows DEGs identified in comparisons of control fruits with those treated with high CO2 on the 1st day and treated with ethylene on the 4th day. Figure 1 summarizes the Gene Ontology (GO) categorization of differentially expressed genes (DEGs) identified in ‘Daebong’ persimmon after high CO2 and ethylene treatments. The GO terms were grouped into three major categories: cellular component, molecular function, and biological process. In the cellular component category, both up- and downregulated genes were predominantly related to the membrane and intracellular anatomical structures under both treatments, accounting for more than 50% of the annotated genes. This indicates that modifications in membrane-associated structures [21] and intracellular membrane decompartmentalization [33] are a key response during deastringency processes in persimmon. Cell membrane permeability changes can facilitate acetaldehyde accumulation in persimmon fruit tissues, thereby promoting tannin insolubilization during deastringency processes [11,34,35]. However, membrane permeability alterations are just one of several factors contributing to acetaldehyde accumulation. The main driver of this accumulation is anaerobic metabolism, which activates PDC and ADH pathways. These physiological changes are reflected in the differential expression of genes categorized by GO analysis. In the cellular component category, both up- and downregulated genes were mainly related to the membrane and intracellular anatomical structures under both treatments. For the molecular function category, a large proportion of DEGs were associated with ion binding and organic cyclic compound binding. Regarding the biological process category, organic substance metabolic process, primary metabolic process, and cellular metabolic process were the most enriched GO terms for both high CO2 and ethylene-treated fruits.
Table 1.
Summary of sequencing data, including raw, trimmed, and mapped reads for ‘Daebong’ persimmon fruits at harvest (control) and after deastringency treatments with high CO2 (1st day) and ethylene (4th day) at 25 °C. It also presents the number of differentially expressed genes (DEGs) identified in comparisons between the control and treated fruits.
Figure 1.
Summary of gene ontology (GO) analysis of differentially expressed genes (DEGs) in ‘Daebong’ persimmon under high CO2 (A–C) and ethylene (D–F) deastringency treatments. The analysis is categorized into cellular component (A,D), molecular function (B,E), and biological process (C,F). In the figure, the outer ring indicates upregulated genes, while the inner ring shows downregulated genes compared with the control. The results are based on comparisons made 1 day after high CO2 treatment and 4 days after ethylene treatment at 25 °C.
3.2. DEGs in the Comparison of High CO2 and Ethylene Treated vs. Control Persimmon Fruit
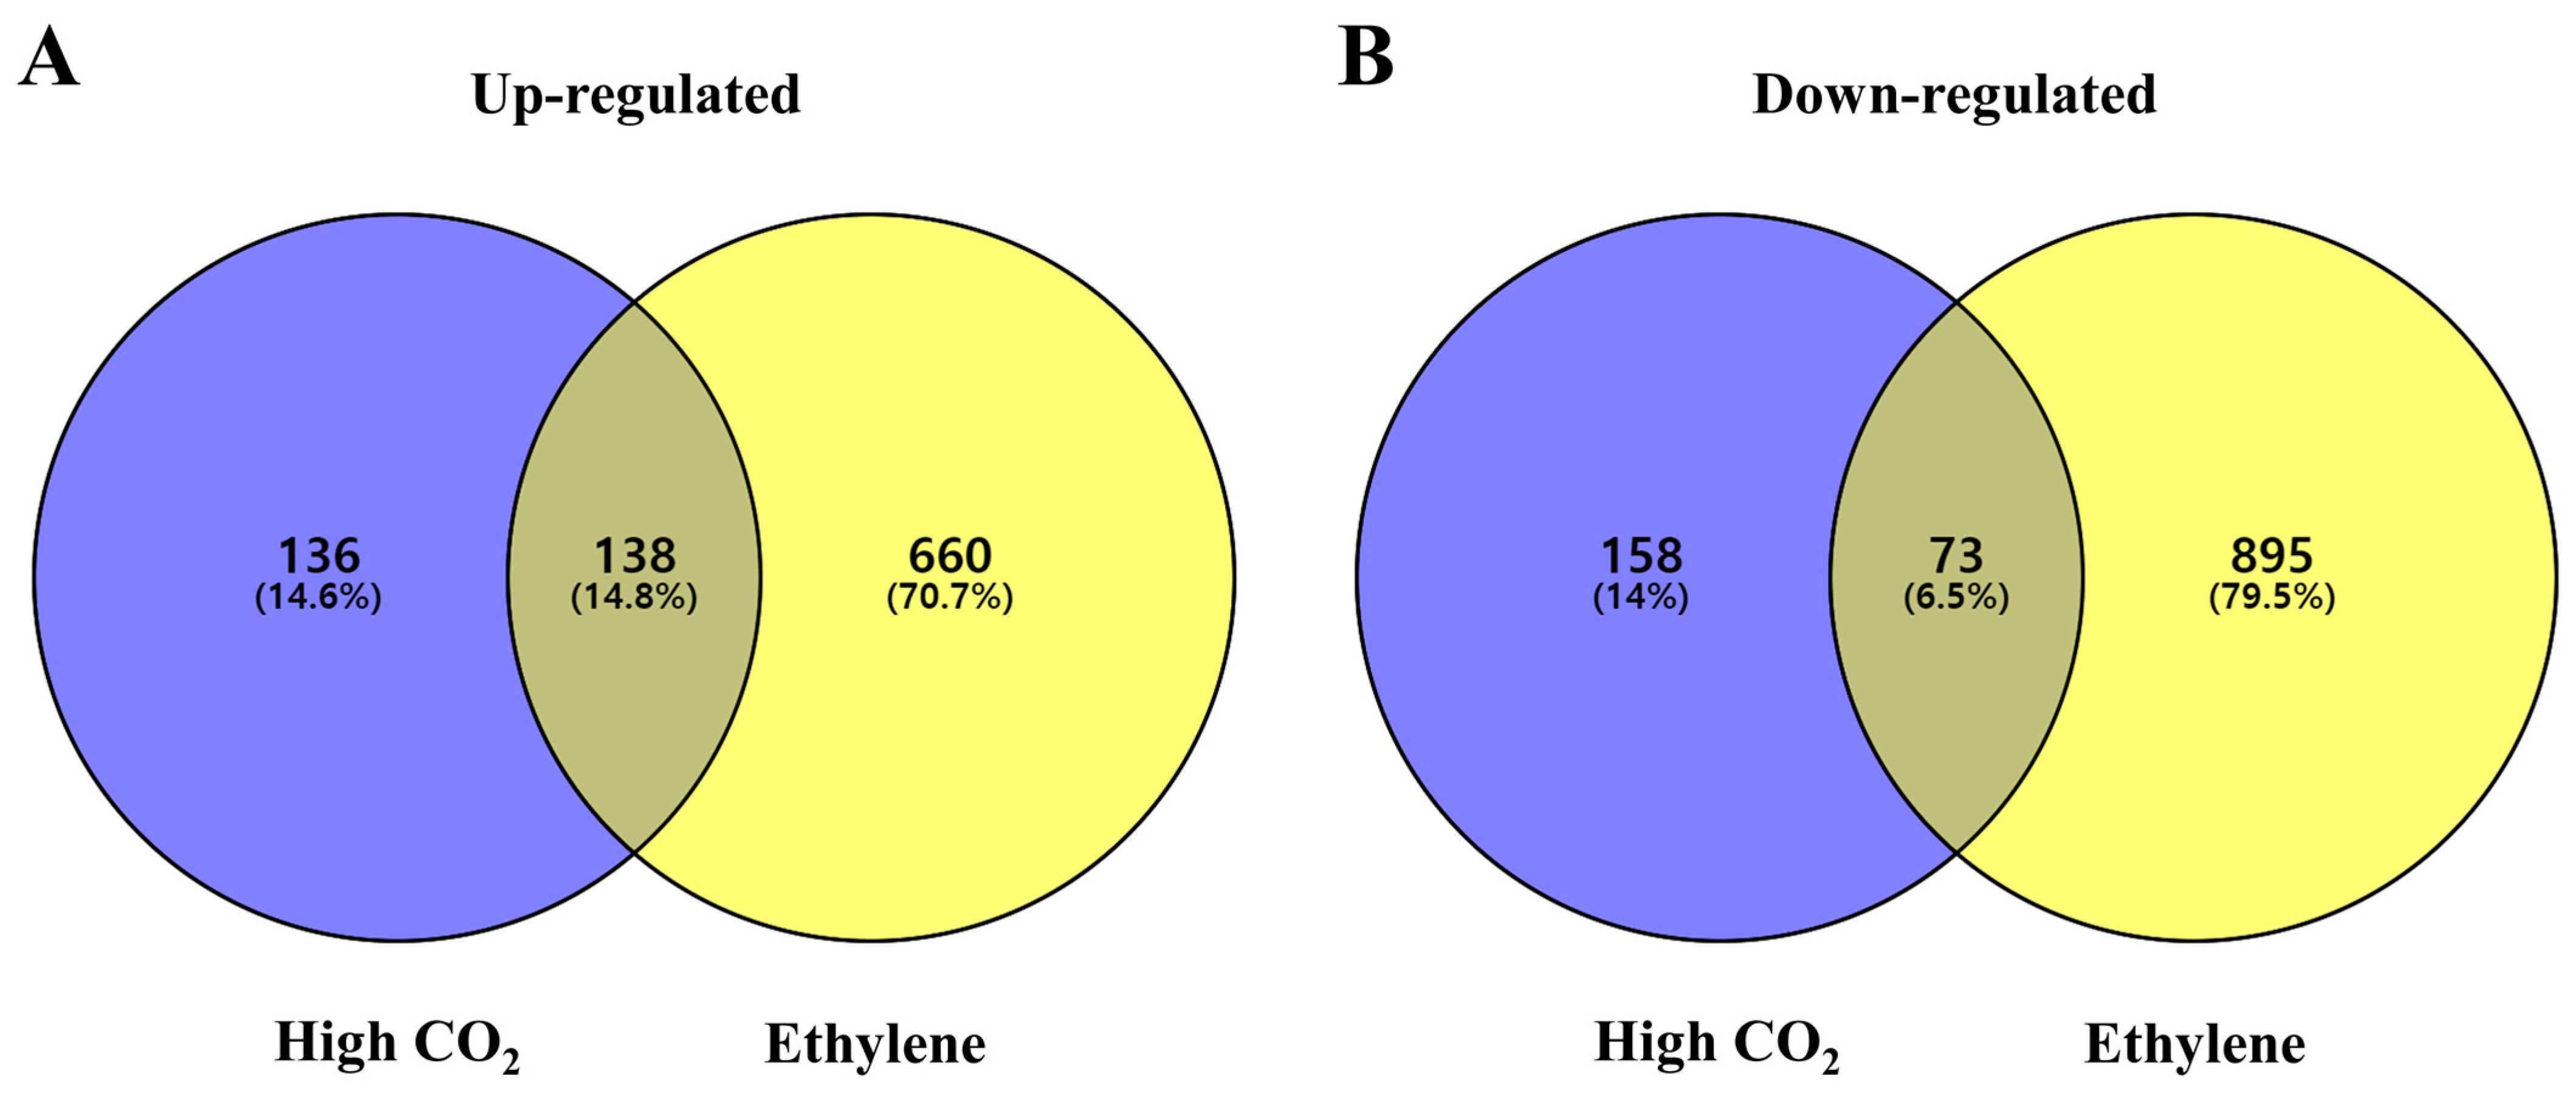
DEGs were identified with a log2 fold change > 2 and p < 0.05 by comparing control fruit with high CO2- and ethylene-treated fruits. A total of 505 and 1766 unigenes were differentially expressed in high CO2- and ethylene-treated fruits, respectively (Table 1). Of these, 274 (29.4%) were upregulated and 231 (20.5%) were downregulated in high CO2-treated fruits, while 798 (85.5%) were upregulated and 968 (86%) were downregulated in ethylene-treated fruits (Table 1). Overall, ethylene treatment induced a larger number of DEGs compared to high CO2 treatment. As summarized in Table 1 and Figure 2, both high CO2 and ethylene treatments resulted in an overall increase in unigene expression compared to the control, with ethylene treatment inducing a larger number of DEGs. Venn diagram analysis revealed that in high CO2-treated fruits, 136 genes (14.6%) were exclusively upregulated and 158 genes (14%) were exclusively downregulated (Figure 2). In ethylene-treated fruits, 660 genes (70.7%) were exclusively upregulated and 895 genes (79.5%) were exclusively downregulated. In addition, 138 genes (14.8%) were commonly upregulated, and 73 genes (6.5%) were commonly downregulated under both treatments (Figure 2). The treatments induced higher unigene expression compared to the control, with ethylene treatment inducing more unigene expression than high CO2 treatment.
Figure 2.
Numbers of commonly and exclusively expressed genes: (A) represents upregulated genes, and (B) represents downregulated genes, based on a log2 fold change greater than 2 and p-value < 0.05, during the comparison of high CO2 (at harvest vs. 1st day under high CO2), ethylene (at harvest vs. 4th day under ethylene in ‘Daebong’ astringent persimmon fruit.
3.3. Soluble Tannin, Total Phenolics, and Genes Related to Deastringency
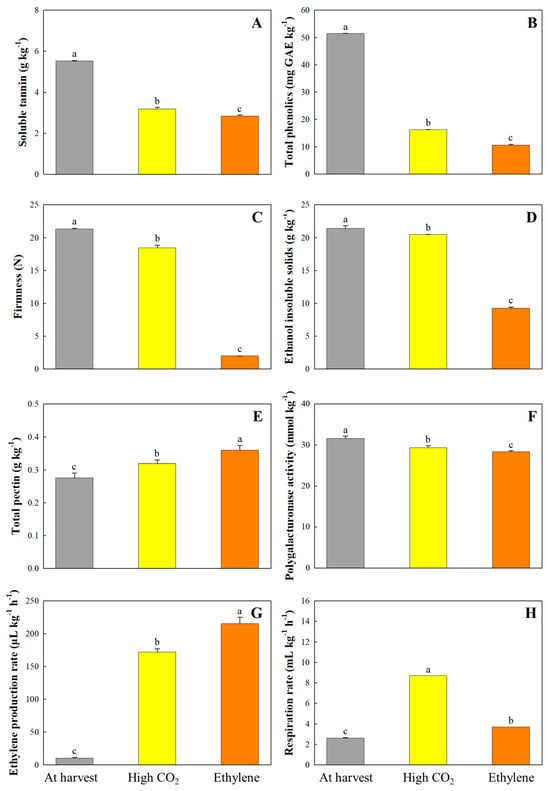
Soluble tannins, a class of high molecular weight polyphenols with numerous hydroxyl groups, are primarily responsible for the astringent sensation in persimmon fruit [2]. In the present study, both high CO2 and ethylene treatments significantly decreased the soluble tannin content in ‘Daebong’ persimmons, thereby enhancing edibility (Figure 3). At harvest, the initial soluble tannin concentration was 5.52 g kg−1. This value declined to 3.18 g kg−1 after one day of high CO2 exposure and further decreased to 2.84 g kg−1 by the fourth day of ethylene treatment (Figure 3). The reduction in tannin content is attributed to acetaldehyde accumulation induced by anaerobic conditions during high CO2 treatment, which promotes the conversion of soluble tannins into insoluble forms, thus effectively mitigating astringency [2]. Meanwhile, Ethylene treatment promotes the transcription of ripening-related genes, including those associated with cell wall degradation and ethylene-responsive transcription factors (ERFs), which subsequently activate downstream genes such as pyruvate decarboxylase (PDC) and alcohol dehydrogenase (ADH). This regulatory cascade facilitates acetaldehyde accumulation and contributes to the polymerization and insolubilization of soluble tannins, thereby inducing a gradual loss of astringency during fruit ripening [21,36,37,38].
Figure 3.
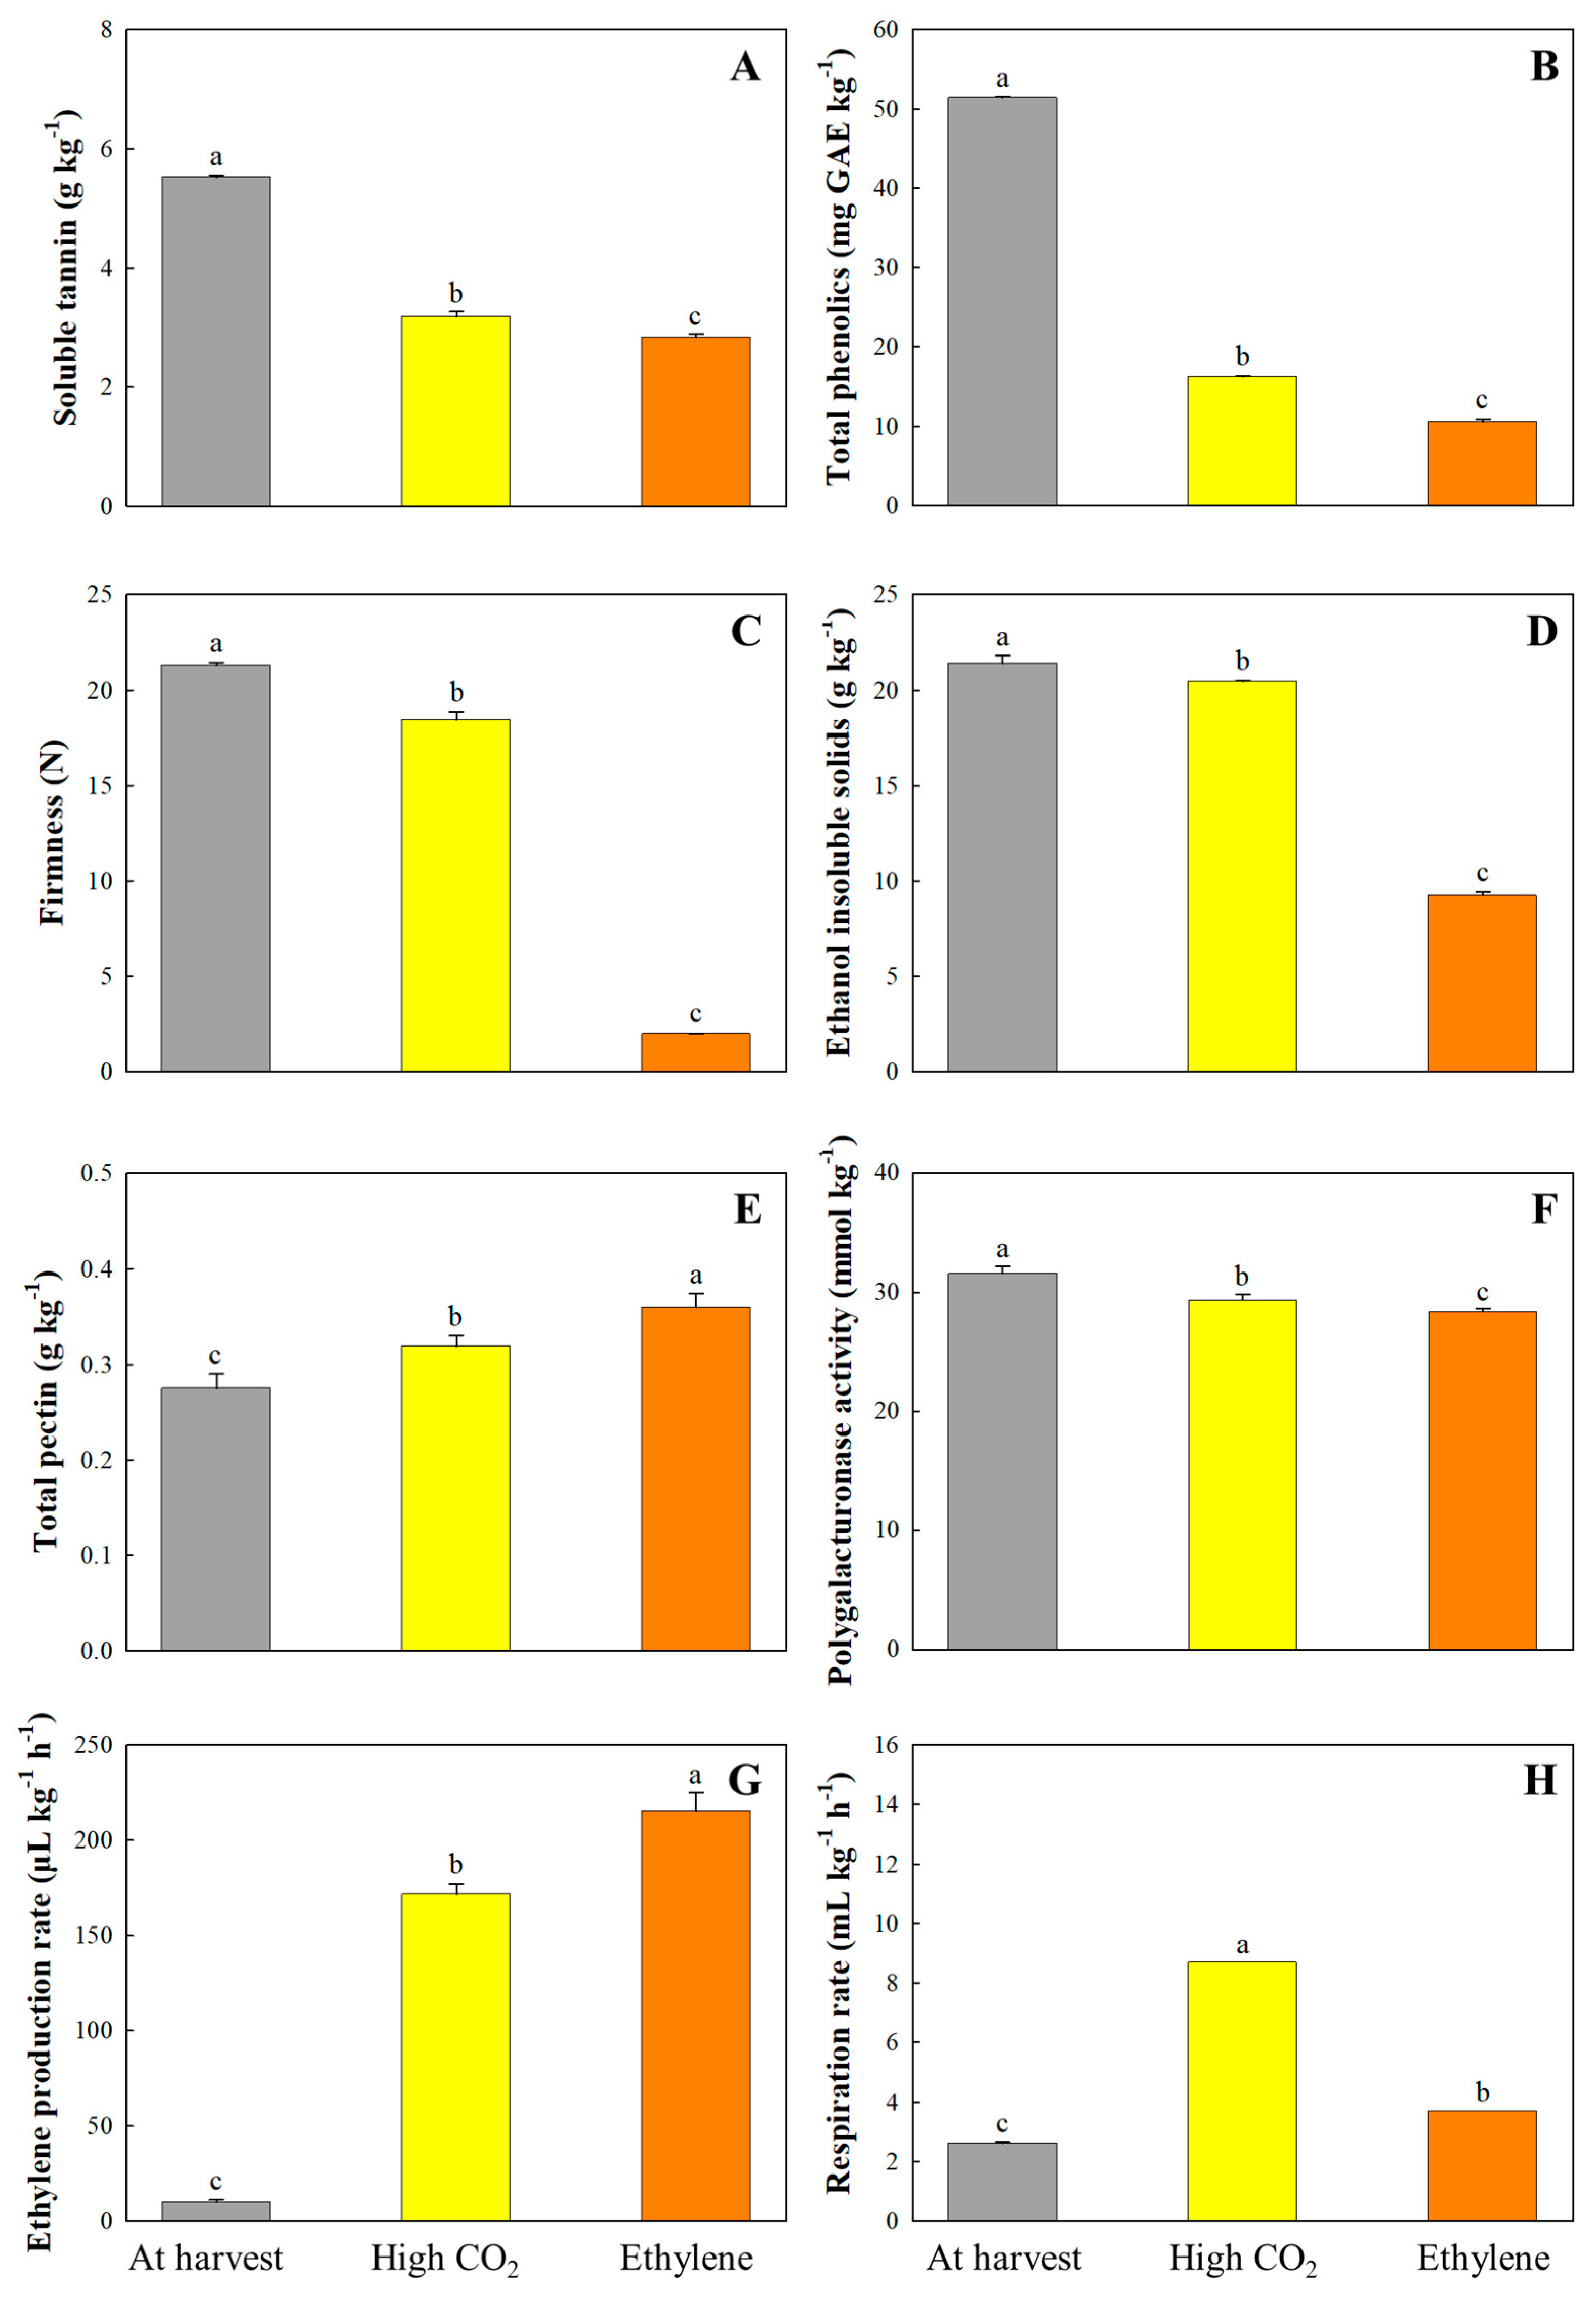
The soluble tannin (A), total phenolics (B), firmness (C), ethanol insoluble solids (EIS) (D), total pectin (E), polygalacturonase (PG) activity (F), ethylene production (G), and respiration rate (H) of the ‘Daebong’ astringent persimmon fruit at harvest, 1 day after high CO2 treatment and 4 days after ethylene treatment at 25 °C. Data are presented as mean ± standard errors (n = 15 for firmness; n = 3 for the other parameters). Different letters on the bars indicate significant differences between treatments at α = 0.05 with Duncan’s mean separation procedure.
The total phenolic content in ‘Daebong’ persimmons was markedly reduced from 5.14 g kg−1 at harvest to 1.62 g kg−1 after one day of high CO2 exposure and continued to decrease to 1.06 g kg−1 by the fourth day following ethylene treatment. Although previous studies have reported a decrease in phenolic and tannin content during ripening or postharvest deastringency [39,40,41], recent comparative analyses suggest that these reductions may follow cultivar-specific regulatory strategies. For instance, high-phenolic cultivars such as ‘Rojo Brillante’ and ‘Rama Forte’ exhibit pronounced declines in tannin levels following CO2 or ethylene exposure, reflecting a rapid transition in their antioxidant and astringency profiles [37,41]. In contrast, other cultivars show more gradual or limited reductions, possibly linked to inherent differences in gene regulation of the phenylpropanoid pathway or polyphenol oxidase activity. Given the substantial decrease in both total phenolics and soluble tannins observed in ‘Daebong’ following deastringency treatment in this study, it is plausible that this cultivar shares a similar regulatory pattern with high-tannin, CO2, or ethylene-sensitive types. Such classification could provide useful insight into tailoring postharvest protocols depending on the biochemical and genetic predisposition of each cultivar.
A similar decline in tannin levels has been reported in ‘Rojo Brillante’ persimmons subjected to postharvest thermal treatment. For example, Cervera-Chiner et al. [31] demonstrated that drying at 40–45 °C reduced tannin content from approximately 30 g kg−1 DW at harvest to below 3 g kg−1 DW, effectively eliminating detectable astringency. This suggests that, regardless of treatment type be it gas exposure or temperature the critical reduction threshold for astringency lies around 3 g kg−1 DW.
To clarify the molecular mechanisms involved in persimmon deastringency, transcriptome profiling was conducted following treatments with high CO2 and ethylene. Both treatments resulted in a significant reduction in soluble tannin content, demonstrating effective deastringency (Figure 3). Additionally, distinct sets of DEGs were identified, with some genes common to both treatments and others specific to each. Among the commonly upregulated genes, sucrose synthase 2-like (SuSy2) and malate synthase, glyoxysomal (MASY) were notably induced (Table 2). Although both genes were upregulated under both CO2 and ethylene treatments, their functional relevance is particularly associated with enhanced glycolytic flux supporting anaerobic metabolism during CO2 treatment. Additionally, 1-aminocyclopropane-1-carboxylate oxidase (ACO) 1, a key enzyme in ethylene biosynthesis, and several ethylene-responsive transcription factors (e.g., ERF12, ERF21, ERF115, ABR1) were upregulated, indicating ethylene signal transduction involvement in both treatments (Table 2). Among the commonly upregulated genes, UGT89B1-like and UGT75C1-like, members of the UDP-glycosyltransferase family, may participate in modifying phenolic compounds through glycosylation. This process could decrease their solubility and contribute to the insolubilization of tannins during the deastringency process (Table 2). Furthermore, the common induction of WRKY11/31, NAC domain-containing proteins, and MYB108 suggests their regulatory involvement in deastringency-related stress responses and phenolic metabolism (Table 2). These transcription factors may act as integrators of hormonal signaling (ethylene, jasmonate) and environmental stress, coordinating the transcriptional reprogramming required for astringency loss. In the CO2-specific transcriptome, several genes involved in anaerobic fermentation and redox metabolism, including ADH 1/3, peroxidase 5-like, and heat shock proteins, were exclusively upregulated. This indicates a metabolic shift towards hypoxic respiration and stress adaptation. Notably, ERF14/26 and WRKY24/46 were also induced specifically under CO2, further supporting their roles in coordinating hypoxia-induced deastringency (Table 3). In contrast, ethylene-specific upregulated genes included phenylalanine ammonia-lyase (PAL) and caffeic acid O-methyltransferase (COMT), which are involved in the phenylpropanoid pathway, potentially enhancing secondary metabolism during ethylene-induced ripening (Table 4). The up-regulation of laccase 5 and polygalacturonase-like genes also implies restructuring of the cell wall and polymerization of phenolic compounds, possibly contributing to insolubilization of soluble tannins (Table 4). Interestingly, 4-coumarate—CoA ligase-like 1 (4CL-like) and beta-amyrin 28-monooxygenase-like, genes linked to lignin and triterpenoid biosynthesis, were commonly downregulated across both treatments, suggesting a suppression of lignification and secondary metabolic branches that may otherwise compete with tannin polymerization processes (Table 2). Overall, these results suggest that CO2 and ethylene treatments both activate distinct and overlapping regulatory networks for soluble tannin insolubilization and phenolic metabolism.
Table 2.
List of DEGs in ‘Daebong’ astringent persimmon cultivar (commonly) in the comparison of high CO2 and ethylene treated vs. control.
Table 3.
List of DEGs in ‘Daebong’ astringent persimmon cultivar (exclusively) in the comparison of high CO2 treated vs. control.
Table 4.
List of DEGs in ‘Daebong’ astringent persimmon cultivar (exclusively) in the comparison of ethylene treated vs. control.
3.4. Firmness, EIS, Total Pectin, PG Activity, and Related Genes
At harvest, the firmness of ‘Daebong’ persimmon fruit was 21.31 N. At the ‘ready to eat’ stage, firmness was significantly retained in high CO2-treated fruit (18.44 N), whereas ethylene-treated fruit showed extensive softening, decreasing to 1.95 N (Figure 3). This pronounced reduction in firmness under ethylene treatment reflects the activation of ripening-associated processes, as previously reported in other climacteric fruits [42,43]. Changes in firmness were paralleled by variations in ethanol-insoluble solids (EIS), which dropped from 21.40 g kg−1 in the control to 9.23 g kg−1 in ethylene-treated fruit. The strong correlation between EIS and texture deterioration suggests that EIS can be a practical biochemical indicator for firmness during persimmon ripening [32]. In contrast, CO2-treated fruit retained higher EIS levels, aligning with the delayed softening. Total pectin content slightly increased during both treatments, reaching 0.32 g kg−1 (CO2) and 0.36 g kg−1 (ethylene), from 0.27 g kg−1 at harvest. Notably, this increase likely reflects pectin solubilization in the early stages of softening, as reported by Taira et al. [44]. However, polygalacturonase (PG) activity—a critical enzyme in pectin depolymerization—was reduced in both treatments, from 31.57 mmol kg−1 in the control to 29.34 mmol kg−1 (CO2) and 28.39 mmol kg−1 (ethylene), suggesting limited enzymatic degradation at the tested stages.
Transcriptomic analysis indicated that these physicochemical changes were closely linked to the expression of genes related to the cell wall. In CO2-treated fruit, notably, the up-regulation of expansin-like A2 and xyloglucan endotransglucosylase/hydrolase (XTH) 23/33 indicates controlled cell wall remodeling without excessive disassembly, thereby contributing to tissue resilience and firmness maintenance. These genes are involved in reversible wall loosening, which enables flexibility while maintaining structural integrity (Table 3). In parallel, peroxidase 5-like and peroxidase 51, which are exclusively upregulated under CO2 treatment, may facilitate the oxidative cross-linking of phenolic compounds within the cell wall matrix (Table 3). This process is believed to enhance structural reinforcement by increasing cell wall rigidity, which improves resistance to softening. Such peroxidase-mediated stiffening mechanisms have been previously implicated in maintaining firmness in climacteric fruits during ripening [21]. On the other hand, the levels of transcripts for several cell wall-degrading enzymes were found to be lower. Pectate lyase 18, expansin A4 (EXPA4), and beta-D-xylosidase were significantly downregulated (Table 3), consistent with the observed suppression of PG activity. In particular, repression of EXPA4, which is typically upregulated during ripening to promote cell wall disassembly, likely plays a key role in restricting tissue softening in CO2-treated fruit. In contrast, ethylene treatment caused increases in transcripts of polygalacturonase-like isoform X2, xyloglucan endotransglucosylase/hydrolase 10 and 11, indicating activation of cell wall modification pathways during softening. However, the softening progression in ‘Daebong’ persimmons seems to require additional post-transcriptional or enzymatic regulation, as transcriptional upregulation alone may not completely account for the observed textural changes. These findings are consistent with previous observations in peach and persimmon, where CO2 treatment suppressed PG activity and preserved firmness through modulation of cell wall-related genes [6,45]. In contrast, ethylene treatment reduced firmness by regulating cell wall–modifying genes [17]. The observed retention of firmness in CO2-treated fruit may thus result from a combination of biochemical stabilization (e.g., EIS maintenance) and transcriptional regulation of cell wall-degrading enzymes. Ethylene-treated fruit, on the other hand, undergoes rapid softening, not necessarily through PG overexpression, but potentially due to the cumulative action of ripening-promoting regulators and ethylene-responsive transcription factors. Collectively, these results highlight the differential regulation of fruit texture by high CO2 and ethylene treatments, underscoring the potential to fine-tune postharvest quality through targeted modulation of associated genes. Both CO2 and ethylene treatments resulted in distinct transcriptional changes associated with cell wall remodeling, which were consistent with observed differences in fruit firmness, EIS, total pectin content, and PG activity. In the ethylene-treated fruits, firmness and EIS values markedly decreased, PG activity showed a slight reduction, and pectin content increased moderately. In contrast, high CO2-treated fruits maintained higher firmness and cellular resistance (Figure 3). At the transcriptional level, ethylene-specific induction of polygalacturonase-like genes (e.g., polygalacturonase At1g48100-like, polygalacturonase) was observed, aligning with the elevated PG activity and enhanced degradation of pectin components (Table 4). These genes are known to catalyze the depolymerization of homogalacturonan, contributing to middle lamella dissolution and tissue softening during fruit ripening and astringency removal. Additionally, the up-regulation of laccase 5 and laccase-15-like may promote phenolic polymerization and cross-linking within the cell wall matrix, further contributing to loss of firmness through structural reorganization.
In contrast, several cell wall biosynthetic and remodeling genes were downregulated in both treatments, particularly in ethylene-treated fruits (Table 2). These include cellulose synthase-like proteins (G3 isoforms), pectinesterase inhibitor 9-like, and beta-xylosidase-like genes, which are essential for cell wall reinforcement and hemicellulose stability. Their suppression suggests attenuation of cell wall renewal and maintenance, potentially favoring wall loosening and cell separation. Notably, expansin-like A2 and xyloglucan endotransglucosylase/hydrolase (XTH) genes were exclusively upregulated under CO2 treatment, indicating a unique remodeling response that may allow controlled loosening of the cell wall without extensive depolymerization (Table 3). Additionally, the CO2-specific up-regulation of peroxidase 5-like and peroxidase 51 may reflect oxidative cross-linking of wall-bound phenolics, contributing to the retention of firmness through wall-strengthening mechanisms. From a hormonal regulation perspective, the up-regulation of ethylene-responsive transcription factors (ERF14/21/115, WIN1-like) and NAC domain-containing proteins (NAC1, NAC2) in both treatments supports their involvement in cell wall-related transcriptional reprogramming (Table 2). In particular, WIN1-like (homologous to Arabidopsis SHINE1), has been implicated in regulating cuticle and cell wall modification genes, potentially acting as a hub for ethylene-mediated wall loosening. Furthermore, the ethylene-specific induction of MYB101, MYB108, and RAV1-like transcription factors may contribute to the transcriptional regulation of wall-degrading enzymes, thereby facilitating cell wall disassembly and the softening process characteristic of ethylene-induced deastringency (Table 4). Under CO2 treatment, the down-regulation of genes such as Expansin A4 (EXPA4), GDSL esterase/lipase (At1g54790-like), and Xyloglucan O-acetyltransferase 4-like indicates a suppression of wall-loosening and pectin-modifying activities (Table 3). This transcriptional pattern likely contributes to the maintenance of cell wall rigidity and firmness during the deastringency process. Collectively, these findings indicate that while both CO2 and ethylene treatments activate cell wall modification pathways essential for deastringency, their regulatory outputs diverge: ethylene promotes active wall degradation and softening, whereas CO2 facilitates controlled remodeling coupled with oxidative wall stabilization, thereby preserving firmness.
3.5. Ethylene Production and Respiration Rates and Related Genes
At the ‘ready-to-eat’ stage, both ethylene production and respiration rates were markedly elevated in ‘Daebong’ persimmon compared to the harvest stage (Figure 3). Ethylene production increased from 9.97 μL kg−1 h−1 at harvest to 171.71 μL kg−1 h−1 after one day of high CO2 treatment and further rose to 215.42 μL kg−1 h−1 following four days of ethylene exposure. Likewise, the respiration rate increased from 2.61 mL kg−1 h−1 at harvest to 8.70 mL kg−1 h−1 in CO2-treated fruit and 3.70 mL kg−1 h−1 in ethylene-treated fruit, respectively. These metabolic responses are likely triggered by external stress signals induced by the deastringency treatments, particularly high CO2, which is known to cause a temporary stimulation of respiratory activity [46]. Despite this initial metabolic activation, high CO2-treated fruits retained firmness, which may be attributed to the repression of cell wall-degrading enzyme activity [45]. Although both metabolic indicators were transiently elevated by CO2 treatment, fruit firmness was largely preserved, especially in comparison to ethylene-treated samples. This paradoxical outcome suggests the presence of transcriptional and metabolic controls that uncouple increased metabolic activity from downstream softening responses. For example, the AP2-like ethylene-responsive transcription factor (At1g16060) was specifically downregulated in CO2-treated fruit (Table 3). As a key regulator of ethylene signaling, this gene controls the expression of cell wall-modifying enzymes, such as expansins and pectinases. Its repression implies a blockade of ethylene-mediated transcriptional cascades, thereby attenuating softening processes even in the presence of ethylene biosynthetic activity. Moreover, the up-regulation of mitochondrial aspartate aminotransferase (AAT) may reflect a metabolic shift toward amino acid interconversion, functioning as a buffer against excess respiratory flux and redox imbalance. In contrast, the down-regulation of pyrophosphate-energized vacuolar membrane proton pump suggests a possible reduction in vacuolar acidification and energy-dependent solute transport, which could restrain enzymatic activities involved in cell wall disassembly. Collectively, these molecular adjustments underscore that the maintenance of firmness under CO2 treatment is not merely due to suppressed ethylene biosynthesis, but rather due to targeted inhibition of ethylene signaling pathways and selective repression of respiration-linked softening mechanisms.
Genes involved in ethylene biosynthesis and signaling were exclusively upregulated under ethylene treatment. Notably, 1-aminocyclopropane-1-carboxylate synthase (ACS), a key rate-limiting enzyme in ethylene biosynthesis, was strongly induced, providing a direct molecular explanation for the observed ethylene surge (Table 4). In addition, the up-regulation of EIN3-binding F-box protein 1-like and ethylene-overproduction protein 1—key components of the ethylene signal transduction cascade—suggests enhanced downstream transcriptional activation of ethylene-responsive genes. Multiple AP2/ERF family transcription factors, including ERF061, ERF113-like, ERF008-like, RAP2-1-like, and RAP2-7-like, were also upregulated, indicating a robust activation of ethylene-mediated transcriptional networks that likely regulate cell wall-degrading enzymes such as polygalacturonases and pectinases (Table 4). This transcriptional reprogramming is aligned with the accelerated softening observed in ethylene-treated fruit. Furthermore, genes associated with respiration and energy metabolism were specifically induced. These include pyruvate decarboxylase 1-like, ATP-dependent 6-phosphofructokinase 4, mitochondrial phosphate carrier protein 3, and respiratory burst oxidase homolog A-like, which are integral to glycolysis, mitochondrial ATP synthesis, and redox regulation (Table 4). Their induction supports the notion that ethylene treatment stimulates energy-demanding processes during ripening.
3.6. Antioxidant Activities and Stress-Related Genes
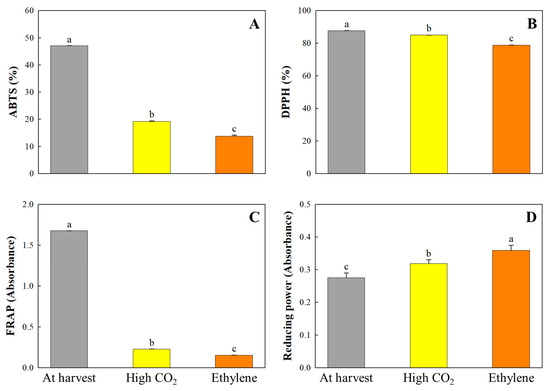
Significant reductions in antioxidant activity were observed in ‘Daebong’ persimmons after both high CO2 and ethylene deastringency treatments, evaluated using ABTS, DPPH, FRAP, and reducing power assays. Notably, ABTS scavenging activity declined from 47.07% at harvest to 19.18% after CO2 treatment and further to 13.75% under ethylene treatment (Figure 4), indicating that ethylene induces greater oxidative deterioration. Despite overall declines, CO2-treated fruits consistently retained higher antioxidant activities than ethylene-treated counterparts, suggesting treatment-specific modulation of stress and redox responses. These trends paralleled changes in soluble tannins and total phenolic content, reinforcing their role as key contributors to the antioxidant profile, as previously reported by Katsube et al. [47] and Denev and Yordanov [40].
Figure 4.
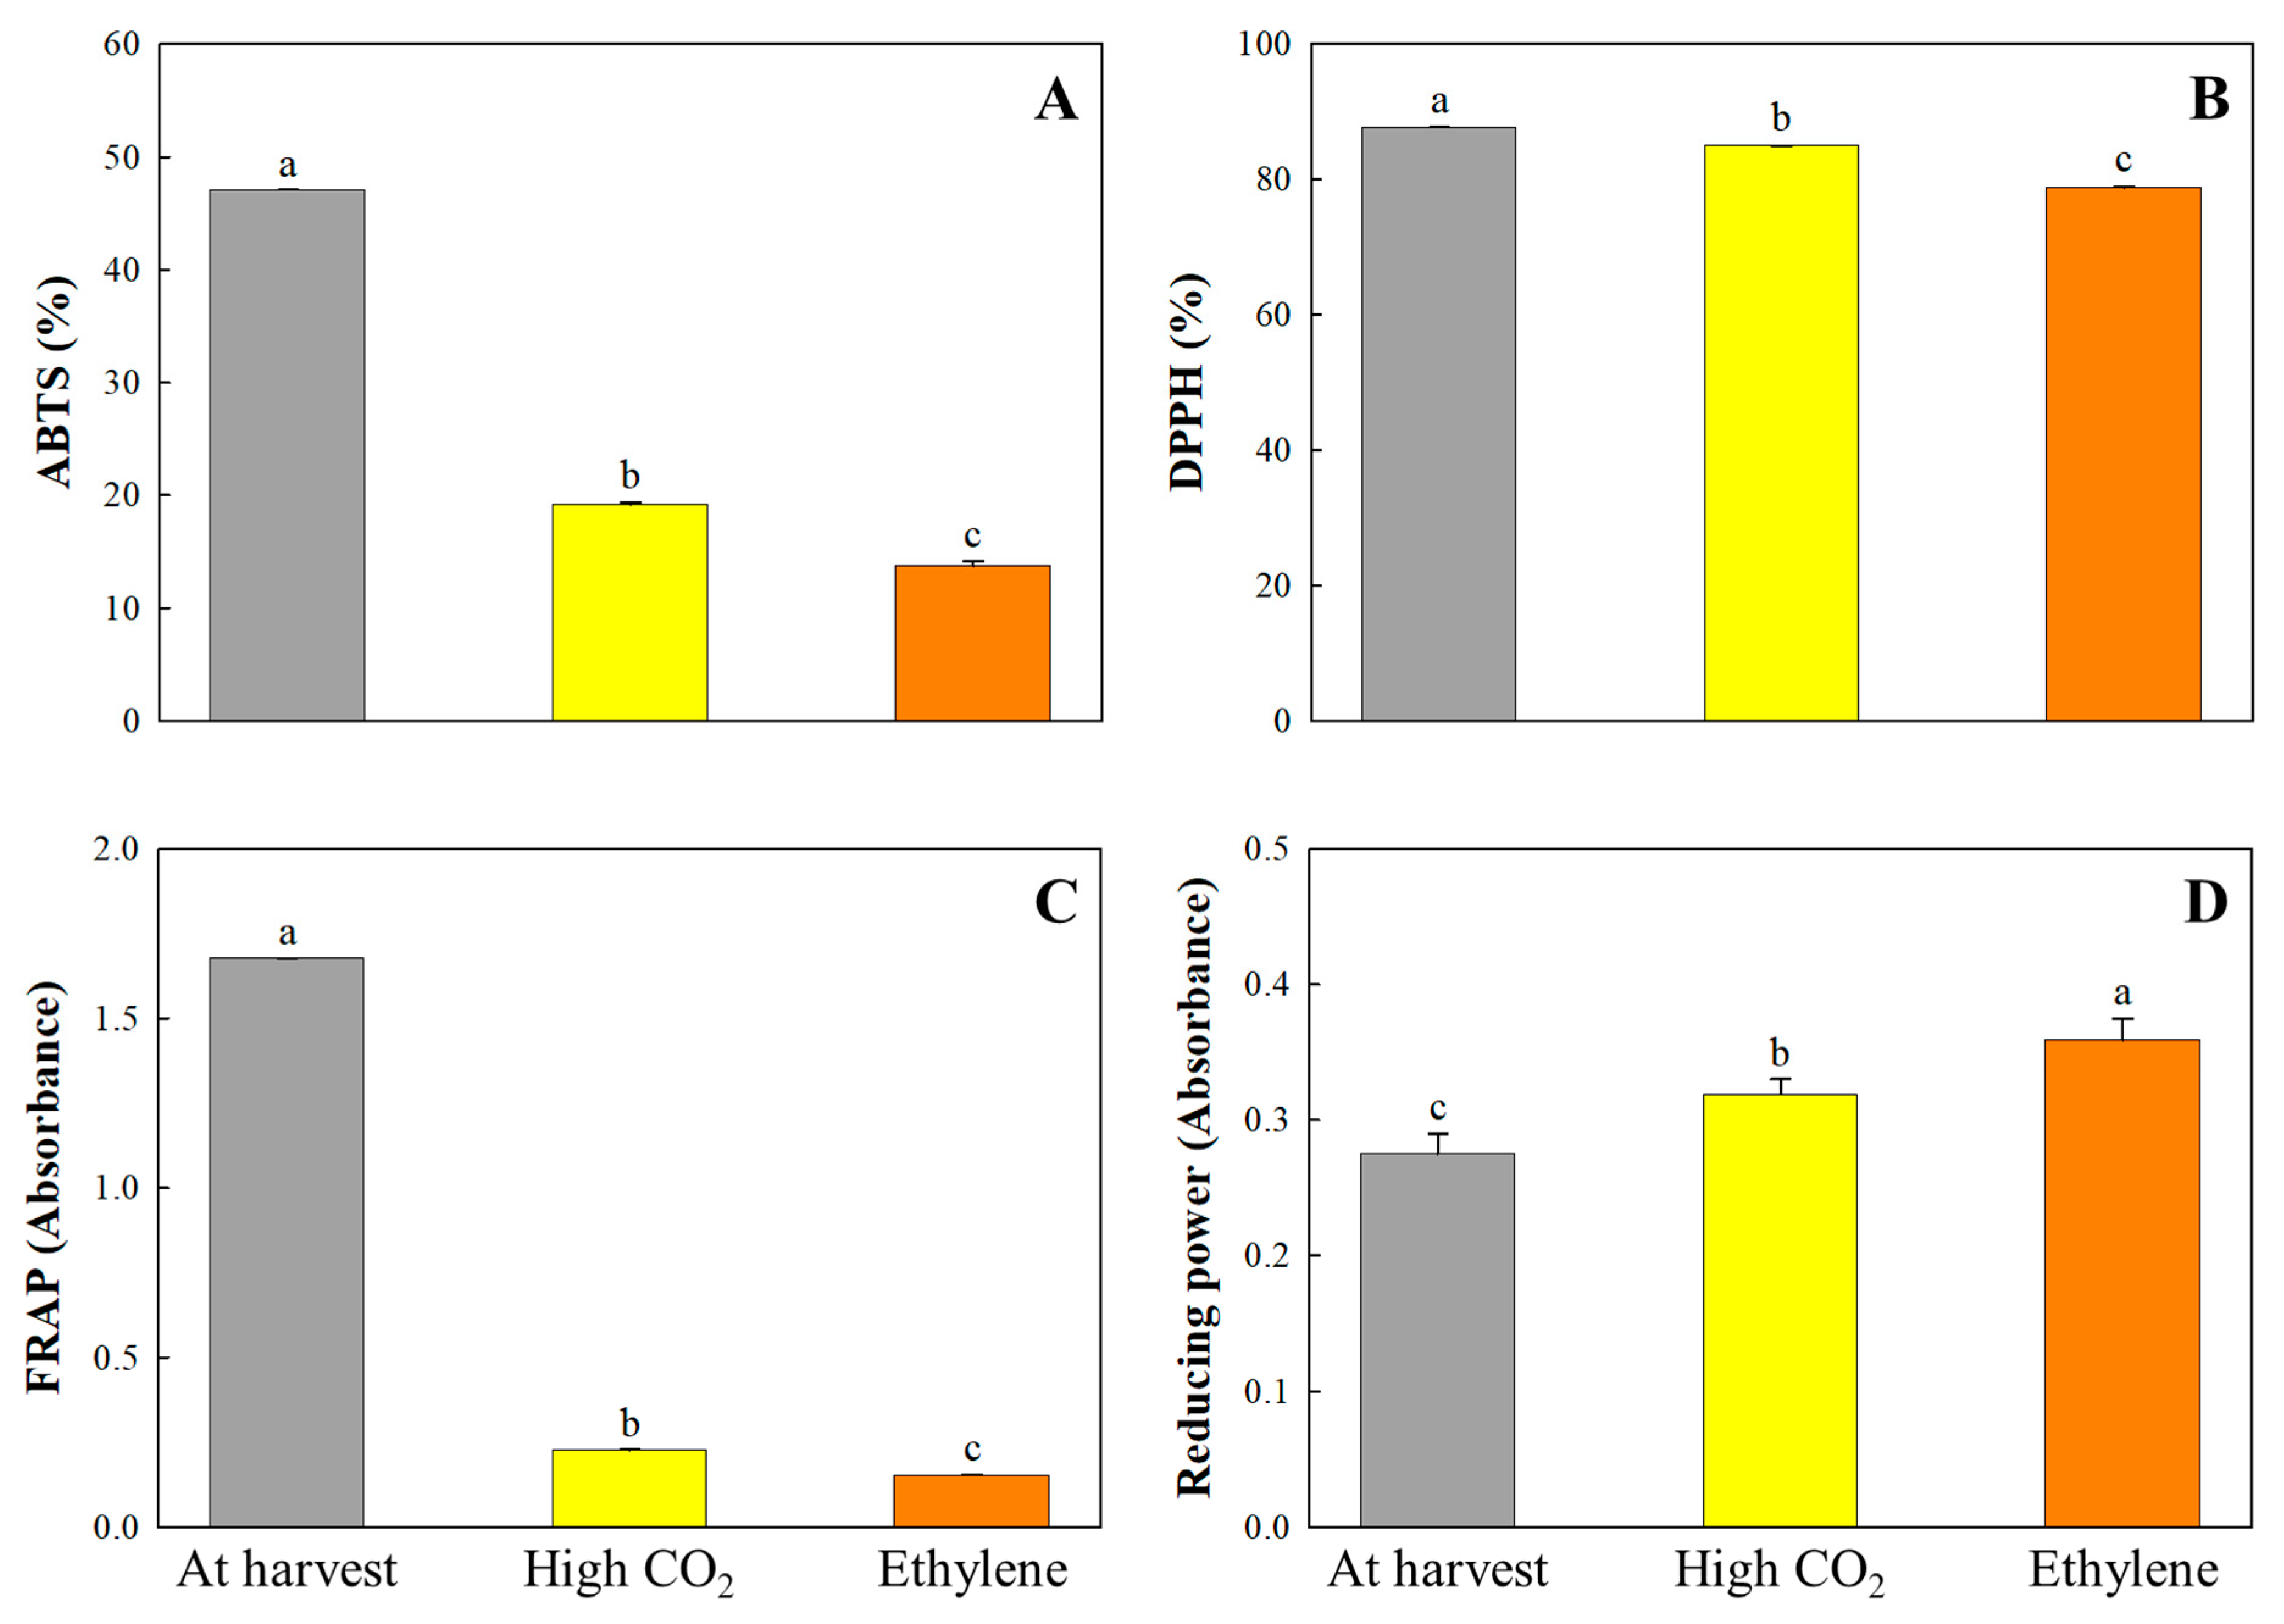
Trolox-equivalent antioxidant capacity (ABTS) (A), DPPH (2,2-di-phenyl-1-picrylhydrazyl) radical scavenging capacity (B), ferric-reducing antioxidant power (FRAP) (C), and reducing power (D) of the ‘Daebong’ astringent persimmon fruit at harvest, 1 day after high CO2 treatment and 4 days after ethylene treatment at 25 °C. Data are presented as mean ± standard errors (n = 3). Different letters on the bars indicate significant differences between treatments at α = 0.05 with Duncan’s mean separation procedure.
Transcriptomic results showed that high CO2 treatment significantly upregulated several genes related to oxidative stress. For example, glutathione S-transferase U17-like (GSTU17) and other GST isoforms were clearly upregulated under CO2 (Table 3), indicating increased detoxification of reactive oxygen species (ROS). The upregulation of peroxidase 5-like, peroxidase 51, and alcohol dehydrogenase 1 and 3 further indicates activation of enzymatic scavenging systems that reduce lipid peroxidation and cellular damage (Table 3). Heat shock proteins (HSPs) such as HSP70, 22 kDa HSP, and several small HSPs were exclusively induced, demonstrating that CO2 triggered a broad cytoprotective response to maintain protein stability under hypoxic stress (Table 3). Moreover, the activation of WRKY and NAC transcription factors—key regulators of abiotic stress and redox homeostasis—suggests a coordinated transcriptional response to maintain cellular stability. The presence of universal stress protein A (USP-A) and jasmonate-induced oxygenase (JOX2) indicates hormonal interactions between jasmonate and ethylene, thereby enhancing defense responses. These molecular adaptations suggest that antioxidant activity remains partially preserved during CO2 treatment, despite the metabolic stress. In contrast, ethylene treatment failed to elicit a comparable stress-mitigating response. While several ethylene-responsive transcription factors were induced, the genes directly related to ROS detoxification and antioxidant defense were notably underrepresented or even suppressed For example, the down-regulation of lipoxygenase (LOX2-1) and peroxidase 12-like (POD5) in response under ethylene (Table 4) indicates reduced ROS signaling and control of lipid peroxidation, which may lead to the observed decrease in antioxidant activity. Furthermore, the limited expression of heat shock proteins (HSPs) and glutathione S-transferases (GSTs) in ethylene-treated samples underscores the treatment’s reduced ability to maintain cellular redox balance during the ripening process. These findings suggest that high CO2 treatment induces a more comprehensive and effective oxidative stress response than ethylene, resulting in improved preservation of antioxidant function and metabolic resilience during deastringency. The transcriptomic results indicate that hypoxia-induced stress under CO2 enhances protective gene expression, offering the dual benefits of astringency removal and retention of nutritional quality.
3.7. Color Changes, Overall Sensory Quality, and the Related Genes
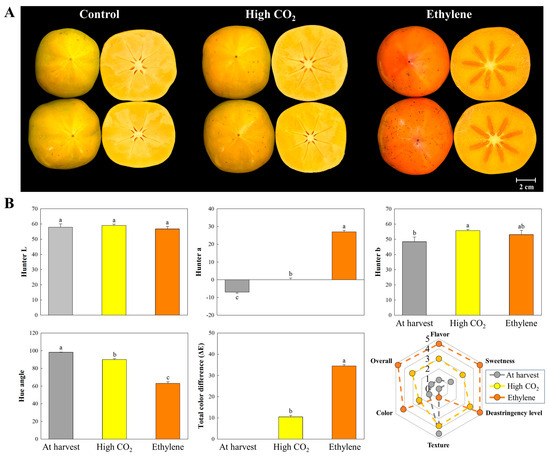
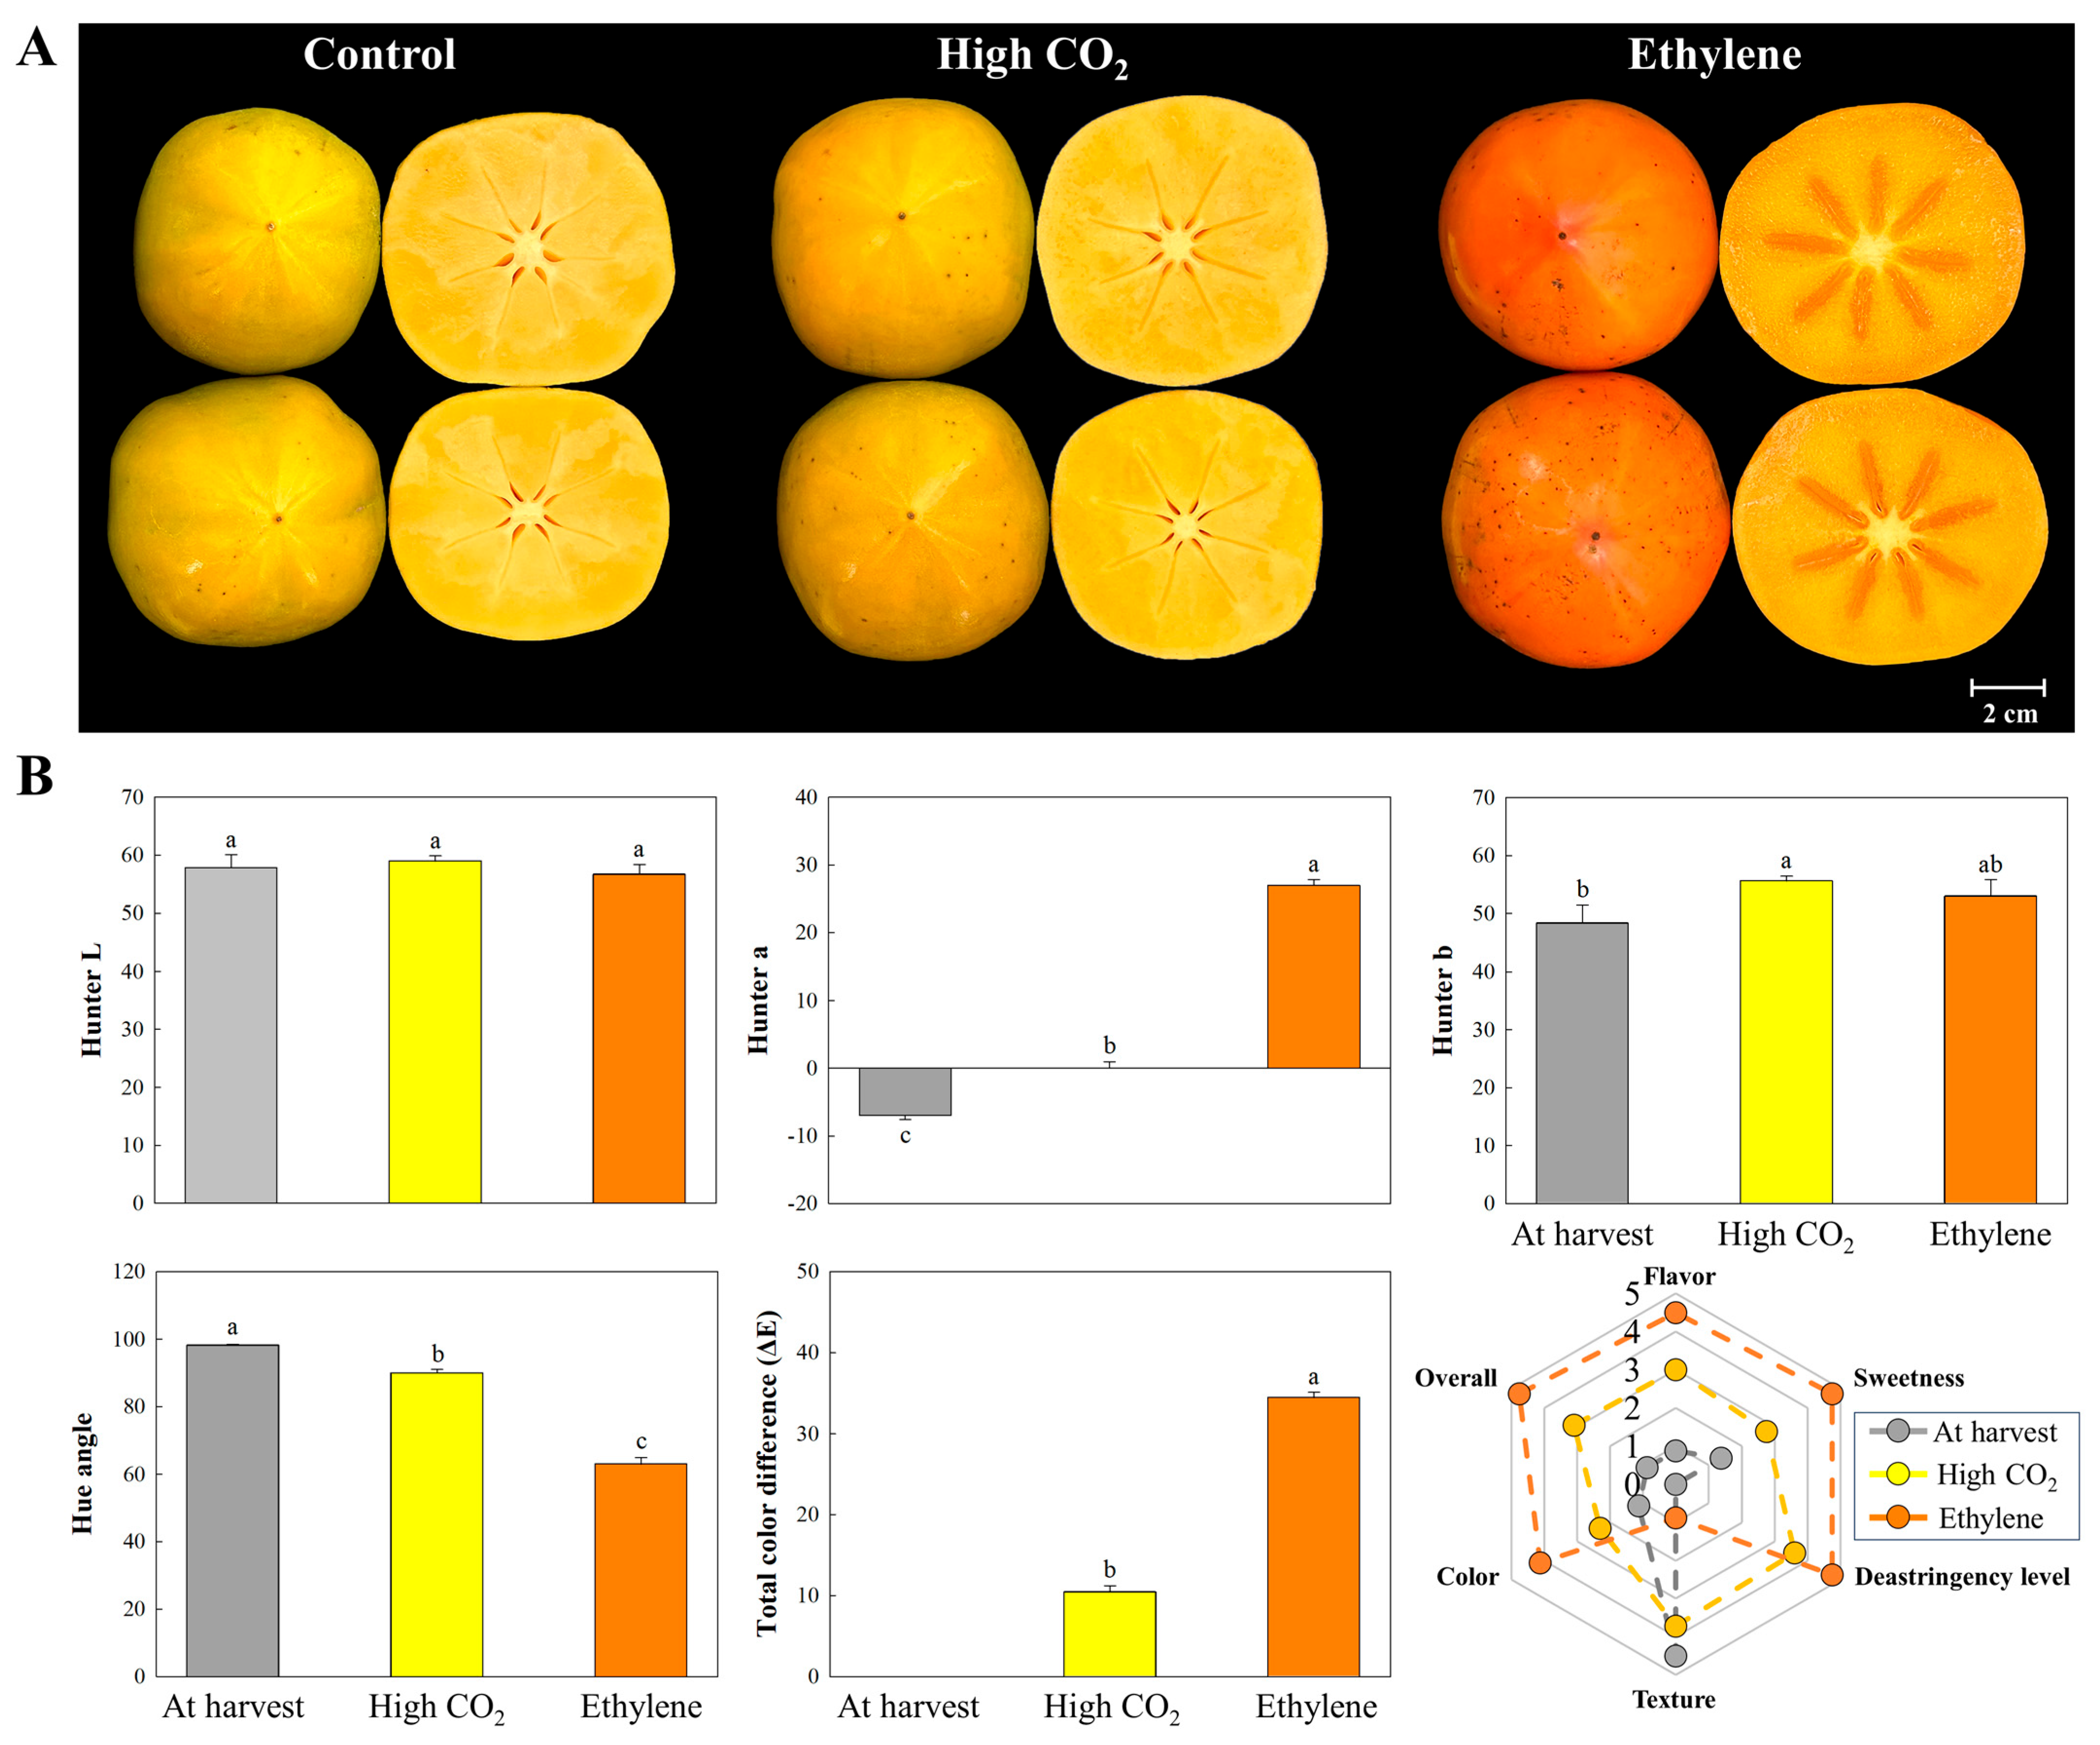
At the ready-to-eat stage, fruits treated with ethylene showed a significantly greater total color difference (ΔE = 34.45) compared to those treated with CO2 (ΔE = 10.44), indicating more advanced ripening and external pigmentation (Figure 5). In ethylene-treated fruit, the overall sensory quality score significantly increased from 0.9 at harvest to 4.75 by day 4, while CO2-treated fruit reached a moderate score of 3.1 on day 1. These findings indicate that ethylene not only improves visual qualities but also increases palatability, likely by reducing soluble tannins and significantly softening, as previously reported by Choi et al. [32]. In contrast, CO2 treatment moderately enhanced color and flavor while preserving firmness, underscoring its role in extending postharvest shelf life.
Figure 5.
Representative photos (A), color parameters (hunter L, a, b values, hue angle, total color difference), and sensory evaluation (B) of ‘Daebong’ astringent persimmon fruit at harvest, 1 day after deastringency treatment with high CO2, and 3 days after deastringency treatment with ethylene at 25 °C. Data are presented as means ± standard errors (n = 15 for color values; n = 10 for sensory evaluation). Different letters on the bars indicate significant differences between treatments at α = 0.05 with Duncan’s mean separation procedure.
Transcriptomic profiling revealed specific regulatory mechanisms related to the treatment that underlies these phenotypic outcomes. In fruit treated with ethylene, genes related to pigment biosynthesis and the formation of volatile compounds were significantly upregulated. Specifically, 9-cis-epoxycarotenoid dioxygenase (NCED2), which catalyzes the oxidative cleavage of carotenoids and contributes to both ABA biosynthesis and color change, was strongly induced. Likewise, Phenylalanine ammonia-lyase (PAL), a key enzyme in the phenylpropanoid pathway, was upregulated, which supports the production of flavonoid precursors that affect both color and taste. Additionally, alcohol acyltransferase 9 and monooxygenase 2-like, which are involved in the biosynthesis of esters and aroma compounds, were upregulated. This indicates an enhancement of fruit flavor and volatile profiles. The activation of these metabolic pathways corresponds with the high sensory acceptance observed in ethylene-treated fruit.
In contrast, the fruit treated with CO2 showed a more controlled transcriptional response, indicating a strategic adjustment of secondary metabolism and structural maintenance instead of accelerating ripening (Table 3). Notably, protein TIFY 9-like and jasmonate-induced oxygenase 1-like isoform X1, exclusively upregulated under CO2 treatment, suggest involvement of the jasmonate signaling pathway, which is known to modulate stress tolerance and may indirectly influence flavor and firmness retention during postharvest treatment. Moreover, the induction of expansin-like A2 and wall-associated receptor kinase-like 10 isoform X5 suggests a regulated cell wall remodeling process, which may facilitate essential but slight changes needed for moderate color development without affecting fruit integrity. Furthermore, universal stress protein A-like protein and glutathione S-transferase U17-like isoform X1 were upregulated, suggesting activation of redox balancing and antioxidant defense systems that could preserve pigment stability and prevent excessive tissue softening under hypoxic CO2 conditions. These expression patterns indicate that high CO2 treatment promotes a unique transcriptional adjustment aimed at maintaining texture and extending shelf life while allowing limited quality enhancement.
Overall, these transcriptional dynamics suggest that ethylene enhances consumer-preferred attributes by activating biosynthetic genes related to color and flavor, while high CO2 preserves structural integrity and influences flavor through the stabilization of secondary metabolites. These differing strategies provide complementary methods for optimizing persimmon postharvest quality based on market needs.
3.8. Partial Least Squares-Discriminant and Correlation Analysis
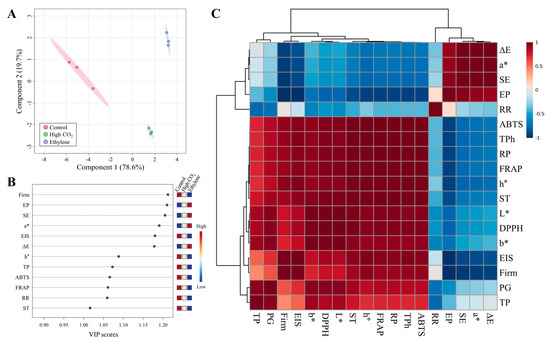
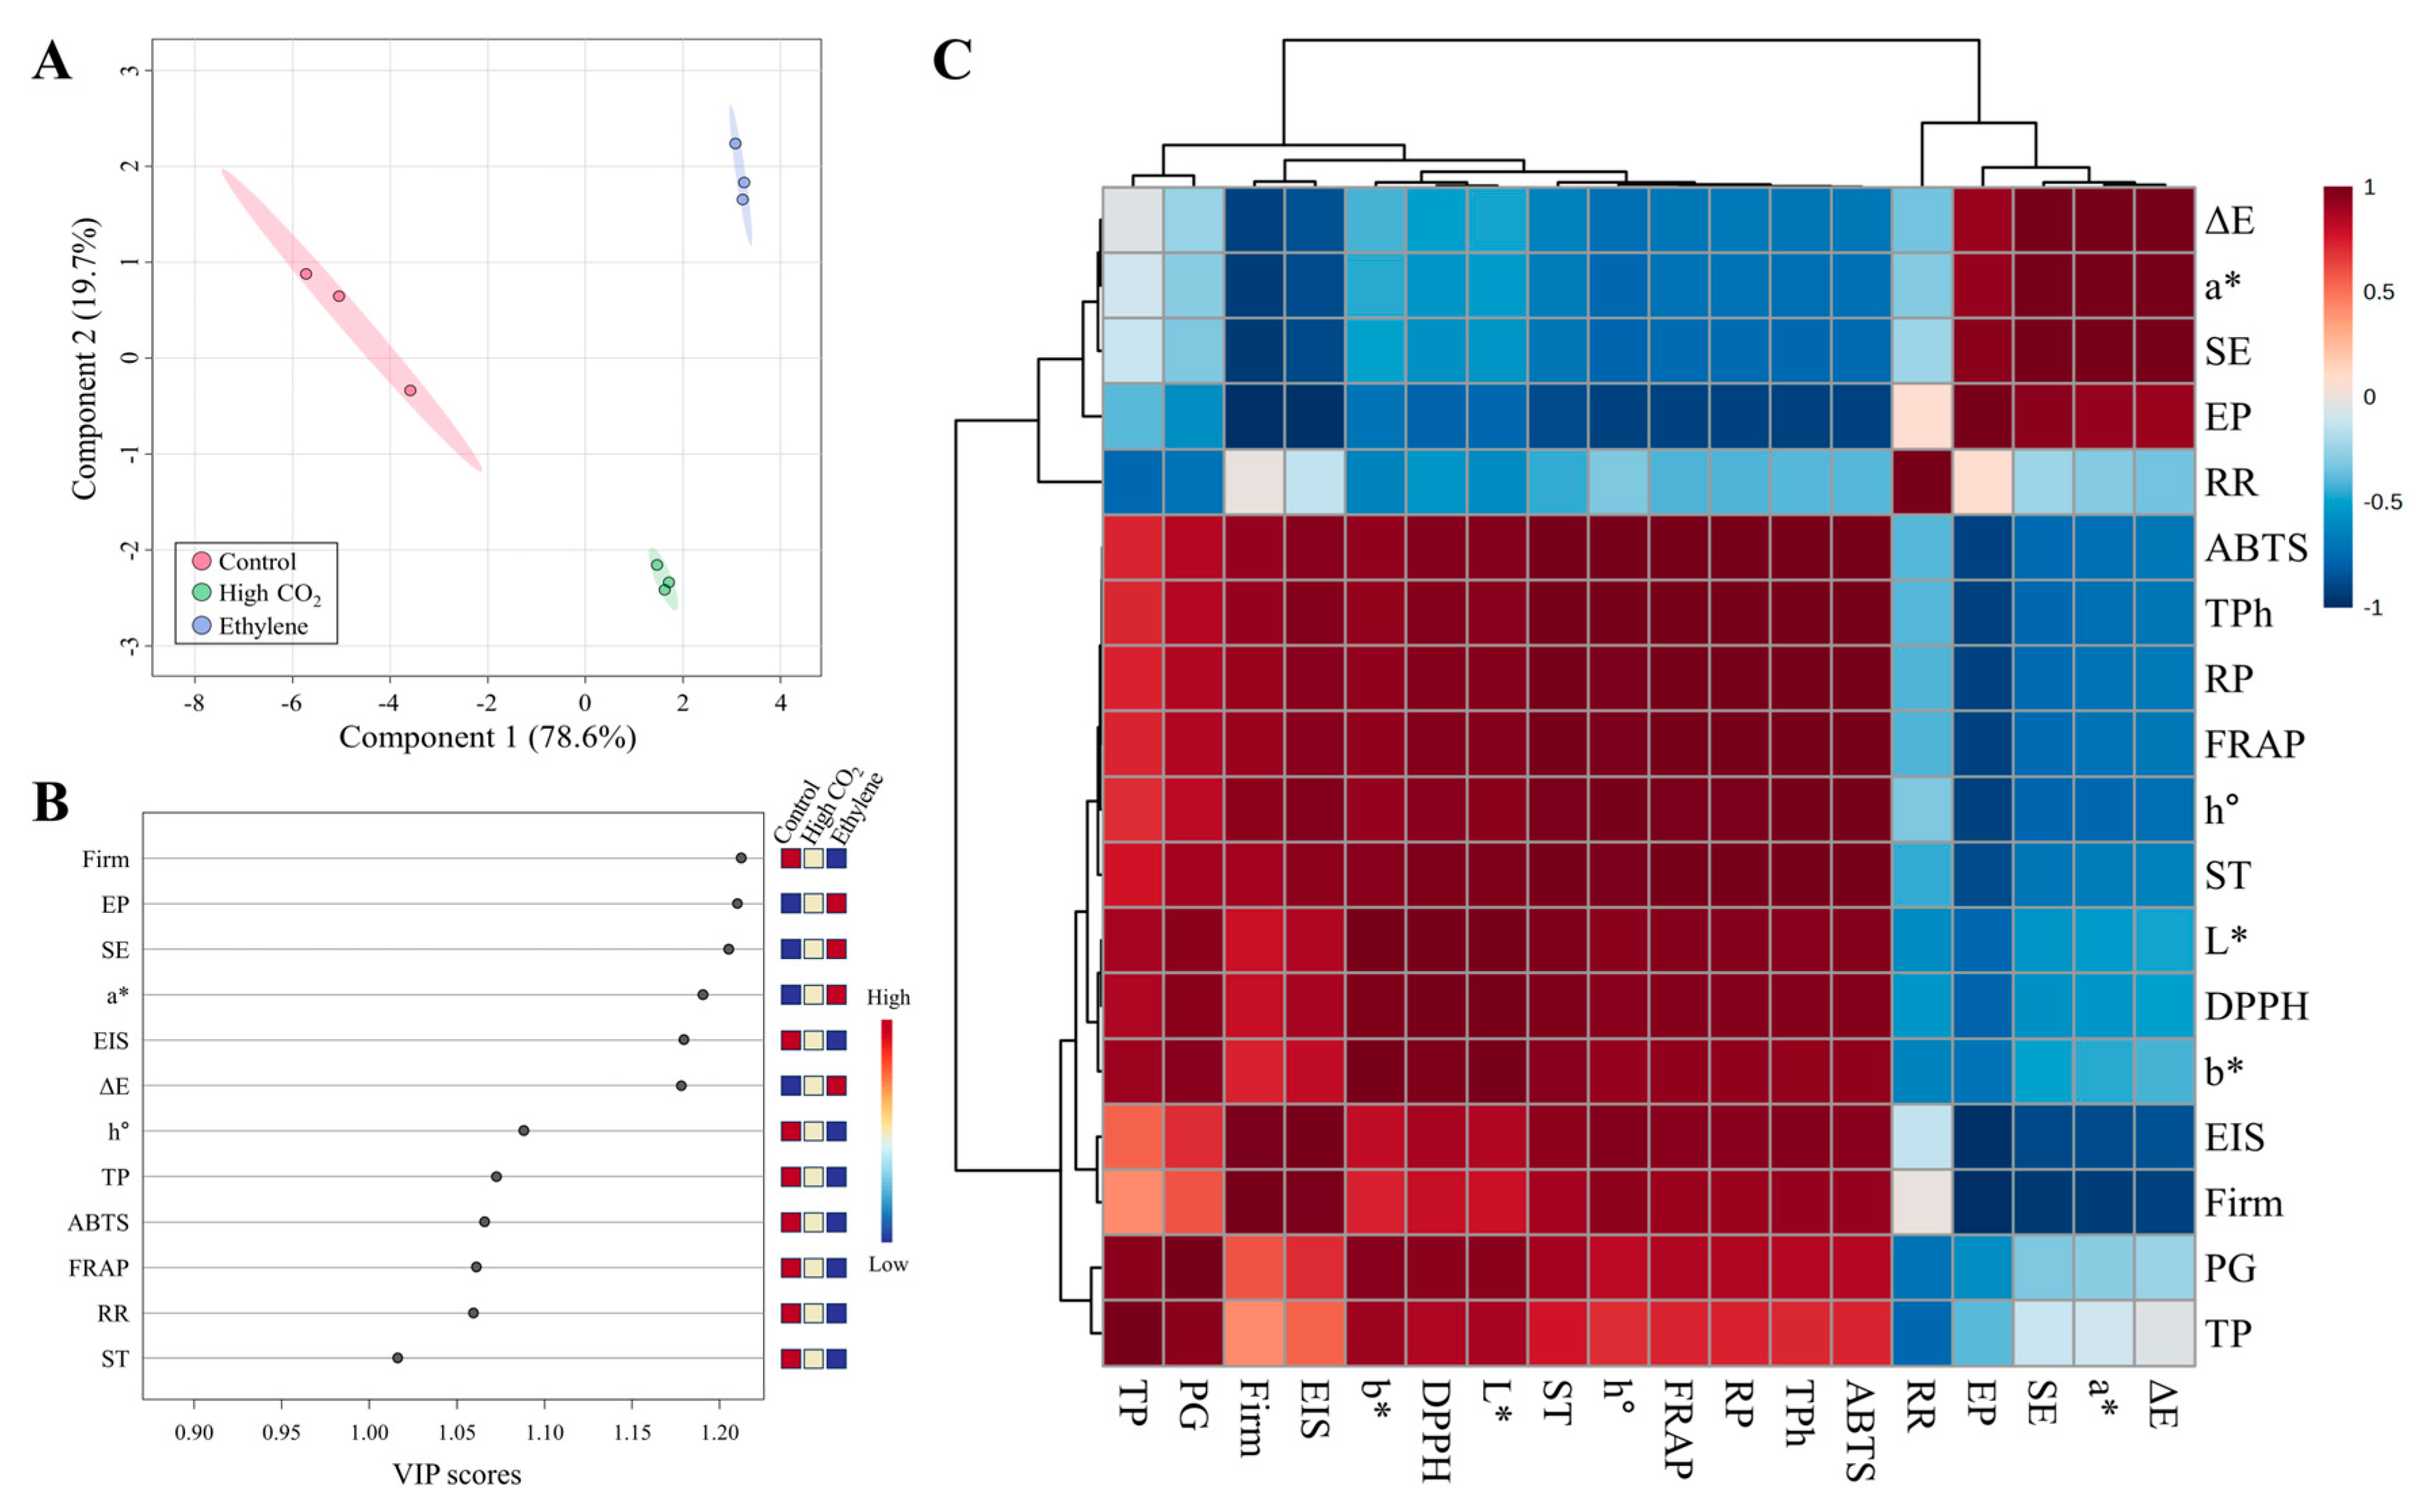
The Partial least squares-discriminant (PLS-DA) score plot (Figure 6A) clearly distinguished the control, high CO2, and ethylene treatment groups along Component 1 (78.6% of the total variance) and Component 2 (10.7%). This separation reflects pronounced differences in quality attributes among the treatments, with both high CO2 and ethylene groups distinctly segregated from the control. Such clustering strongly suggests that the postharvest treatments induced specific metabolic and color changes associated with degreening processes.
Figure 6.
Partial least squares-discriminant analysis (PLS-DA) scores plot (A); variable importance in projection (VIP) scores plot (B); correlation heatmap (C) of the observed parameters in ‘Daebong’ astringent persimmon fruit at harvest, 1 day after deastringency treatment with high CO2, and 3 days after deastringency treatment with ethylene at 25 °C. ΔE, a*, SE, EP, RR, ABTS, TPh, RP, FRAP, h°, ST, L*, DPPH, b*, EIS, RR, Firm, PG, and, TP, represent color difference, Hunter a value, sensory evaluation, ethylene production rate, respiration rate, 2,2′-azino-bis(3-ethylbenzothiazoline-6-sulfonic acid), total phenols, reducing power, ferric reducing antioxidant power, hue angle, soluble tannin, Hunter L value, α-diphenyl-β-picrylhydrazyl, Hunter b value, ethanol insoluble solids, firmness, polygalacturonate activity, and total pectin, respectively. The heatmap’s red and blue boxes show positive and negative correlations.
VIP score analysis (Figure 6B) revealed that the most influential variables for treatment discrimination, in descending order, were firmness, ethylene production rate (EP), sensory evaluation (SE), a*, ethanol insoluble solids (EIS), ΔE, h°, and total phenolics (TP). These parameters are closely related to tissue integrity, pigment changes, and the accumulation of antioxidant compounds, serving as critical indicators for assessing quality retention during deastringency. Firmness and EIS, in particular, were strongly associated with quality maintenance in the CO2-treated group, supporting previous findings that CO2 treatment preserves firmness by suppressing cell wall degradation [45].
Pearson’s correlation analysis (Figure 6C) demonstrated a remarkably strong positive correlation between firmness and EIS (r = 0.990), highlighting a close link between cellular structural integrity and physical firmness. Firmness also showed strong positive correlations with color stability (h°, r = 0.939) and TP (r = 0.920), while exhibiting strong negative correlations with maturity-associated parameters such as EP (r = −0.982) and a* (r = −0.935). These patterns indicate that firmness loss is directly associated with accelerated color shifts and surface property changes, indicative of ripening.
Antioxidant activity was found to be tightly linked with total phenolics. TP was almost perfectly correlated with FRAP (r = 0.9997) and ABTS (r = 0.9998), while soluble tannin content also showed strong correlations with FRAP (r = 0.9966) and ABTS (r = 0.9968). These findings suggest that antioxidant capacity is primarily determined by the phenolic fraction, particularly soluble tannins. Regarding colorimetric indices, a* was highly correlated with total color change (ΔE, r = 0.998) and surface color uniformity (SE, r = 0.994), while b* was strongly correlated with lightness (L*, r = 0.994). Collectively, these results provide mechanistic insights into the maintenance of color stability in high CO2-treated fruit and the rapid pigment alterations observed in the ethylene-treated group. Moreover, the correlation patterns identified in Figure 6A–C offer a quantitative basis for developing non-destructive predictive models and designing targeted quality management strategies during storage and distribution.
4. Conclusions
This study showed that both high CO2 and ethylene treatments effectively reduced the soluble tannin content in ‘Daebong’ persimmons, aiding in deastringency. However, the effects on fruit quality traits, especially firmness, varied significantly. Fruits treated with high levels of CO2 maintained their firmness despite increased ethylene production and respiration rates. This suggests a role for transcriptional repression of ethylene signaling (AP2-like ERFs), reduced vacuolar transport activity, and enhanced antioxidant defense mechanisms. The activation of hypoxia-related genes and ROS-scavenging enzymes under CO2 treatment indicates an adaptive strategy for stress mitigation that maintains structural and biochemical stability. In contrast, treatment with ethylene initiated a broader transcriptional reprogramming, including the up-regulation of ACS, polygalacturonase, ERF genes, and genes related to energy metabolism. Collectively, these changes promoted rapid softening, development of pigments, and enhancement of sensory qualities. These varying responses underscore the intricate relationship between hormonal signaling, cell wall metabolism, and oxidative stress pathways during the deastringency of persimmons. The transcriptomic and biochemical responses specific to the cultivar described in this study offer a detailed molecular framework for enhancing postharvest treatment protocols for astringent persimmons. Using high CO2 treatment to remove astringency while preserving firmness and antioxidant capacity offers an effective strategy for maintaining postharvest quality in PCA-type cultivars like ‘Daebong’.
Author Contributions
M.W.B.: Conceptualization, Investigation, Data curation, Formal analysis. S.T.: Investigation, Supervision, Writing—original draft, Writing—review and editing. S.M.C.: Investigation, Data curation. D.P.: Writing—review and editing. C.S.J.: Conceptualization, Investigation, Supervision, Writing—review and editing. All authors have read and agreed to the published version of the manuscript.
Funding
This study was supported by the National Research Foundation of Korea (NRF) grant funded by the Korea government (MIST) (RS-2023-00240947) and by the BK21 FOUR project.
Data Availability Statement
The original contributions presented in this study are included in the article. Further inquiries can be directed to the corresponding authors.
Conflicts of Interest
The authors declare no conflicts of interest.
Correction Statement
This article has been republished with a minor correction to the Data Availability Statement. This change does not affect the scientific content of the article.
References
- FAOSTAT. Food and Agriculture Organization of the United Nations Statistics Division. Available online: http://www.fao.org/home/en (accessed on 1 May 2024).
- Baek, M.W.; Choi, H.R.; Hwang, I.G.; Tilahun, S.; Jeong, C.S. Prediction of tannin content and quality parameters in astringent persimmons from visible and near-infrared spectroscopy. Front. Plant Sci. 2023, 14, 1260644. [Google Scholar] [CrossRef] [Scilit]
- Park, D.S.; Tilahun, S.; Heo, J.Y.; Jeong, C.S. Quality and expression of ethylene response genes of ‘Daebong’ persimmon fruit during ripening at different temperatures. Postharvest Biol. Technol. 2017, 133, 57–63. [Google Scholar] [CrossRef] [Scilit]
- Joo, O.-S.; Kang, S.-T.; Jeong, C.-H.; Lim, J.-W.; Park, Y.-G.; Cho, K.-M. Manufacturing of the enhances antioxidative wine using a ripe daebong persimmon (Dispyros kaki L.). J. Appl. Biol. Chem. 2011, 54, 126–134. [Google Scholar] [CrossRef] [Scilit]
- Sato, A.; Yamada, M. Persimmon breeding in Japan for pollination-constant non-astringent (PCNA) type with marker-assisted selection. Breed. Sci. 2016, 66, 60–68. [Google Scholar] [CrossRef] [Scilit]
- Zhu, Q.-G.; Xu, Y.; Yang, Y.; Guan, C.-F.; Zhang, Q.-Y.; Huang, J.-W.; Grierson, D.; Chen, K.-S.; Gong, B.-C.; Yin, X.-R. The persimmon (Diospyros oleifera Cheng) genome provides new insights into the inheritance of astringency and ancestral evolution. Hortic. Res. 2019, 6, 138. [Google Scholar] [CrossRef] [Scilit]
- Das, P.R.; Eun, J.-B. Removal of astringency in persimmon fruits (Diospyros kaki) subjected to different freezing temperature treatments. J. Food Sci. Technol. 2021, 58, 3154–3163. [Google Scholar] [CrossRef] [Scilit]
- Chung, H.-S.; Kim, H.-S.; Lee, Y.-G.; Seong, J.-H. Effect of deastringency treatment of intact persimmon fruits on the quality of fresh-cut persimmons. Food Chem. 2015, 166, 192–197. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Ozdemir, A.E.; Candir, E.; Toplu, C.; Yildiz, E. Effect of hot water treatment on astringency removal in persimmon cultivars. Int. J. Fruit Sci. 2020, 20 (Suppl. S2), S557–S569. [Google Scholar] [CrossRef] [Scilit]
- Cortés, V.; Rodríguez, A.; Blasco, J.; Rey, B.; Besada, C.; Cubero, S.; Salvador, A.; Talens, P.; Aleixos, N. Prediction of the level of astringency in persimmon using visible and near-infrared spectroscopy. J. Food Eng. 2017, 204, 27–37. [Google Scholar] [CrossRef] [Scilit]
- Tanaka, T.; Matsuo, Y.; Saito, Y. Solubility of tannins and preparation of oil-soluble derivatives. J. Oleo Sci. 2018, 67, 1179–1187. [Google Scholar] [CrossRef] [Scilit]
- Eram, M.S.; Ma, K. Decarboxylation of pyruvate to acetaldehyde for ethanol production by hyperthermophiles. Biomolecules 2013, 3, 578–596. [Google Scholar] [CrossRef] [Scilit]
- Waarde, A. Alcoholic fermentation in multicellular organisms. Physiol. Zool. 1991, 64, 895–920. [Google Scholar] [CrossRef] [Scilit]
- Kou, J.; Wei, C.; Zhao, Z.; Guan, J.; Wang, W. Effects of ethylene and 1-methylcyclopropene treatments on physiological changes and ripening-related gene expression of ‘Mopan’ persimmon fruit during storage. Postharvest Biol. Technol. 2020, 166, 111185. [Google Scholar] [CrossRef] [Scilit]
- Shimomura, M. Ripening control with ethylene and ethephon on a rapid-deastringency system in persimmon fruits. Int. Persimmon Symp. 1996, 436, 215–234. [Google Scholar] [CrossRef] [Scilit]
- Kato, K. Astringency removal and ripening in persimmons treated with ethanol and ethylene. Hortic. Sci. 1990, 25, 205–207. [Google Scholar] [CrossRef] [Scilit]
- He, Y.; Xue, J.; Li, H.; Han, S.; Jiao, J.; Rao, J. Ethylene response factors regulate ethylene biosynthesis and cell wall modification in persimmon (Diospyros kaki L.) fruit during ripening. Postharvest Biol. Technol. 2020, 168, 111255. [Google Scholar] [CrossRef] [Scilit]
- Park, D.S.; Tilahun, S.; Park, K.C.; Choi, I.Y.; Jeong, C.S. Transcriptome analysis of astringent ‘Cheongdo-Bansi’ persimmon fruit treated with ethylene for removal of astringency. Postharvest Biol. Technol. 2019, 150, 52–59. [Google Scholar] [CrossRef] [Scilit]
- Nishiyama, S.; Onoue, N.; Kono, A.; Sato, A.; Yonemori, K.; Tao, R. Characterization of a gene regulatory network underlying astringency loss in persimmon fruit. Planta 2018, 247, 733–743. [Google Scholar] [CrossRef] [Scilit]
- Ding, Y.; Shen, X.; Ding, Y.; Zhang, P.; Zhu, Q.; Wang, Y.; Zhang, Q.; Luo, Z.; Yang, Y.; Du, X.; et al. A comprehensive transcriptomic and metabolomic map reveals the molecular mechanism of persimmon fruit deastringency upon 40 °C warm water treatment. Postharvest Biol. Technol. 2025, 220, 113313. [Google Scholar] [CrossRef] [Scilit]
- Salvador, A.; Arnal, L.; Besada, C.; Larrea, V.; Quiles, A.; Pérez-Munuera, I. Physiological and structural changes during ripening and deastringency treatment of persimmon fruit cv. ‘Rojo Brillante’. Postharvest Biol. Technol. 2007, 46, 181–188. [Google Scholar] [CrossRef] [Scilit]
- Wu, W.; Wang, M.-M.; Gong, H.; Liu, X.-F.; Guo, D.-L.; Sun, N.-J.; Huang, J.-W.; Zhu, Q.-G.; Chen, K.-S.; Yin, X.-R.; et al. High CO2/hypoxia-induced softening of persimmon fruit is modulated by DkERF8/16 and DkNAC9 complexes. J. Exp. Bot. 2020, 71, 2690–2700. [Google Scholar] [CrossRef] [Scilit]
- Mamrot, J.; Legaie, R.; Ellery, S.J.; Wilson, T.; Seemann, T.; Powell, D.R.; Gardner, D.K.; Walker, D.W.; Temple-Smith, P.; Papenfuss, A.T.; et al. De novo transcriptome assembly for the spiny mouse (Acomys cahirinus). Sci. Rep. 2017, 7, 8996. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bolger, A.M.; Lohse, M.; Usadel, B. Trimmomatic: A flexible trimmer for Illumina sequence data. Bioinformatics 2014, 30, 2114–2120. [Google Scholar] [CrossRef] [Scilit]
- Li, H. Aligning sequence reads, clone sequences and assembly contigs with BWA-MEM. arXiv 2013, arXiv:1303.3997. [Google Scholar] [CrossRef] [Scilit]
- Choi, H.R.; Tilahun, S.; Park, D.S.; Lee, Y.M.; Choi, J.H.; Baek, M.W.; Jeong, C.S. Harvest time affects quality and storability of kiwifruit (Actinidia spp.) Cultivars during long-term cool storage. Sci. Hortic. 2019, 256, 108523. [Google Scholar] [CrossRef] [Scilit]
- Seo, M.H.; Tilahun, S.; Park, D.S.; Melaku, A.; Jeong, C.S. Effect of ripening conditions on the quality and storability of muskmelon (Cucumis melo L.) fruits. J. Hortic. Sci. Technol. 2018, 36, 741–755. [Google Scholar] [CrossRef] [Scilit]
- Tewari, R.; Gupta, M.; Ahmad, F.; Rout, P.K.; Misra, L.; Patwardhan, A.; Vasudeva, R. Extraction, quantification and antioxidant activities of flavonoids, polyphenols and pinitol from wild and cultivated Saraca asoca bark using RP-HPLC-PDA-RI method. Ind. Crop. Prod. 2017, 103, 73–80. [Google Scholar] [CrossRef] [Scilit]
- Baek, M.W.; Choi, H.R.; Solomon, T.; Jeong, C.S.; Lee, O.-H.; Tilahun, S. Preharvest Methyl Jasmonate Treatment Increased the Antioxidant Activity and Glucosinolate Contents of Hydroponically Grown Pak Choi. Antioxidants 2021, 10, 131. [Google Scholar] [CrossRef] [Scilit]
- Choi, Y.-E.; Choi, S.-I.; Han, X.; Men, X.; Jang, G.-W.; Kwon, H.-Y.; Kang, S.-R.; Han, J.-S.; Lee, O.-H. Radical scavenging-linked anti-adipogenic activity of aster scaber ethanolic extract and its bioactive compound. Antioxidants 2020, 9, 1290. [Google Scholar] [CrossRef] [Scilit]
- Cervera-Chiner, L.; Vilhena, N.Q.; Larrea, V.; Moraga, G.; Salvador, A. Influence of temperature on ‘Rojo Brillante’ persimmon drying. Quality characteristics and drying kinetics. LWT 2024, 197, 115902. [Google Scholar] [CrossRef] [Scilit]
- Choi, H.R.; Baek, M.W.; Cheol, L.H.; Jeong, C.S.; Tilahun, S. Changes in metabolites and antioxidant activities of green ‘Hayward’ and gold ‘Haegeum’ kiwifruits during ripening with ethylene treatment. Food Chem. 2022, 384, 132490. [Google Scholar] [CrossRef] [Scilit]
- Sarkhosh, A.; Habibi, F.; Brecht, J.K. Alleviating Astringency in Persimmon Fruit for Enhanced Palatability and Consumer Acceptability: HS1483, 5/2024. EDIS 2024, 3, 1–7. [Google Scholar] [CrossRef] [Scilit]
- Arnal, L.; del Río, M.A. Effect of cold storage and removal astringency on quality of persimmon fruit (Diospyros kaki L.) cv. Rojo Brillante. Food Sci. Technol. Int. 2004, 10, 179–185. [Google Scholar] [CrossRef] [Scilit]
- Tanaka, T.; Takahashi, R.; Kouno, I.; Nonaka, G.-I. Chemical evidence for the de-astringency (insolubilization of tannins) of persimmon fruit. J. Chem. Soc. Perkin Trans. 1994, 1, 3013–3022. [Google Scholar] [CrossRef] [Scilit]
- Zhao, W.; Zheng, M.; Li, X.; Song, K.; Shi, D. Fruit Astringency: Mechanisms, Technologies, and Future Directions. Horticulturae 2025, 11, 699. [Google Scholar] [CrossRef] [Scilit]
- Amorim, C.; Antoniolli, L.R.; Orsi, B.; Kluge, R.A. Advances in metabolism and genetic control of astringency in persimmon (Diospyros kaki Thunb.) fruit: A review. Sci. Hortic. 2023, 308, 111561. [Google Scholar] [CrossRef] [Scilit]
- Tessmer, M.A.; Appezzato-Da-Glória, B.; Kluge, R.A. Astringency in ‘Giombo’ persimmon and its relationship with the harvest time. Rev. Ceres 2016, 63, 646–652. [Google Scholar] [CrossRef] [Scilit]
- Barbosa, M.C.F.; Morais, M.A.S.; Melo, M.F.; Souza, P.A.; Sarmento, J.D.A.; Morais, P.L.D. Maturation and antioxidant activity of ‘Giombo’ and ‘Rama Forte’ persimmons produced in the Brazilian semiarid. Braz. J. Biol. 2024, 84, e276146. [Google Scholar] [CrossRef] [Scilit]
- Denev, P.; Yordanov, A. Total polyphenol, proanthocyanidin and flavonoid content, carbohydrate composition and antioxidant activity of persimmon (Diospyros kaki L.) fruit in relation to cultivar and maturity stage. Bulg. J. Agric. Sci. 2013, 19, 981–988. [Google Scholar]
- Del Bubba, M.; Giordani, E.; Pippucci, L.; Cincinelli, A.; Checchini, L.; Galvan, P. Changes in tannins, ascorbic acid and sugar content in astringent persimmons during on-tree growth and ripening and in response to different postharvest treatments. J. Food Compos. Anal. 2009, 22, 668–677. [Google Scholar] [CrossRef] [Scilit]
- Seymour, G.B.; Østergaard, L.; Chapman, N.H.; Knapp, S.; Martin, C. Fruit development and ripening. Annu. Rev. Plant Biol. 2013, 64, 219–241. [Google Scholar] [CrossRef] [Scilit]
- Giovannoni, J.J. Genetic regulation of fruit development and ripening. Plant Cell 2004, 16 (Suppl. S1), S170–S180. [Google Scholar] [CrossRef] [Scilit]
- Taira, S.; Ono, M.; Matsumoto, N. Reduction of persimmon astringency by complex formation between pectin and tannins. Postharvest Biol. Technol. 1997, 12, 265–271. [Google Scholar] [CrossRef] [Scilit]
- Choi, H.R.; Jeong, M.J.; Baek, M.W.; Choi, J.H.; Lee, H.C.; Jeong, C.S.; Tilahun, S. Transcriptome Analysis of Pre-Storage 1-MCP and High CO2-Treated ‘Madoka’ Peach Fruit Explains the Reduction in Chilling Injury and Improvement of Storage Period by Delaying Ripening. Int. J. Mol. Sci. 2021, 22, 4437. [Google Scholar] [CrossRef] [Scilit]
- Yang, S.F.; Hoffman, N.E. Ethylene biosynthesis and its regulation in higher plants. Annu. Rev. Plant Physiol. 1984, 35, 155–189. [Google Scholar] [CrossRef]
- Katsube, T.; Tabata, H.; Ohta, Y.; Yamasaki, Y.; Anuurad, E.; Shiwaku, K.; Yamane, Y. Screening for antioxidant activity in edible plant products: Comparison of low-density lipoprotein oxidation assay, DPPH radical scavenging assay, and Folin−Ciocalteu assay. J. Agric. Food Chem. 2004, 52, 2391–2396. [Google Scholar] [CrossRef] [Scilit]

Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).