Article

Stress and the City: Body Condition, Blood Parameters, Parasite Load, and Stomach Calorimetry of Rural and Urban European Rabbit Populations

1
Independent Researcher, 14548 Schwielowsee, Germany
2
Department of River Ecology and Conservation, Senckenberg Research Institute and Natural History Museum Frankfurt, Clamecystr. 12, 63571 Gelnhausen, Germany
3
The Fraunhofer Institute for Cell Therapy and Immunology, Perlickstraße 1, 04103 Leipzig, Germany
4
Frankfurt University Hospital, Theodor-Stern-Kai 7, 60596 Frankfurt am Main, Germany
5
Independent Researcher, 63225 Langen, Germany
6
Department of Ecology and Evolution, Goethe University Frankfurt, Biologicum, Campus Riedberg, Max-von-Laue-Str. 13, 60438 Frankfurt am Main, Germany
7
State Museum of Natural History Stuttgart, Department of Zoology, Museum am Löwentor, Rosenstein 1, 70191 Stuttgart, Germany
8
Independent Researcher, 10629 Berlin, Germany
*
Author to whom correspondence should be addressed.
Submission received: 10 April 2025 / Revised: 21 May 2025 / Accepted: 4 June 2025 / Published: 16 June 2025

Simple Summary

The presence of wildlife in cities used to be a rare phenomenon, but this has clearly changed over the last decades. More and more animals, such as foxes, wild boars, or wild rabbits, are thriving in urban areas due to food abundance, a milder microclimate, and less predation pressure. However, wild animals in urban areas face other threats, such as traffic, pollution, or permanent disturbance by humans. In this study, we asked whether urban rabbit populations live an overall healthier life than their rural conspecifics. We compared age, weight, physiological health parameters, as well as the caloric energy value of the stomach content of 39 urban and 34 rural rabbits. Furthermore, we collected rabbit fecal samples from rural, suburban, and urban areas in order to assess the parasite load in rabbit latrines. While rural rabbits exhibit higher overall body mass and fat reserves, urban rabbits show increased internal organ weights and altered blood parameters. Parasite prevalence and diversity were generally higher in rural rabbits, though specific parasites were more common in urban populations. Our study suggests that living in the city could lead to physiological adaptations to urban stressors such as the chronic exposure to pollutants.

Abstract

(1) Background: We combined physiological and morphological data of the European rabbit (Oryctolagus cuniculus) to provide insights into the question of how urbanization affects the health of urban wildlife populations. (2) Methods: We dissected 39 urban and 34 rural wild rabbits in order to compare organ weights, as well as stomach contents. Furthermore, we collected blood and fecal samples. (3) Results: Rural rabbits had a significantly longer body and a higher body weight as well as more fat tissue around their kidneys compared to urban rabbits. In contrast, the stomach, the intestines, the liver, the lung, and the brain of urban rabbits were significantly heavier. The amount of hematocrit, hemoglobin, and the mean corpuscular volume was significantly higher in urban rabbits. The caloric energy content of the stomach was comparable between rural and urban rabbits and was merely influenced by the season being higher in autumn. Rural rabbits had an overall higher mean parasite index compared to urban rabbits. (4) Conclusions: The results of our study allow for a deeper understanding of how density-dependent (e.g., transmission of diseases) and density-independent factors (e.g., food quality) influence the health status and life history traits of urban wildlife populations compared to their rural counterparts.

1. Introduction

1.1. The Anthropogenic Impact on Urban Wildlife

Species that initially evolved under natural conditions with respective selection factors now live in areas of high anthropogenic influences, i.e., within the urban environment. As a consequence of the higher and more consistent availability of food within the city, urban wildlife shows shifts in their diets and feeding habits, e.g., urban mammals and birds learn how to use anthropogenic food sources [1,2,3]. Several studies suggest that by taking advantage of these human-induced food sources (e.g., litter, intentional feeding), many urban birds and mammals are able to meet their caloric intake requirements much faster compared to their rural conspecifics (in black bears, Ursus americanus [4]; Eurasian red squirrel, Sciurius vulgaris [5]; or birds [6,7]; but see Eurasian coot, Fulica atra [8,9] for contrasting results).
On the one hand, the higher availability of food sources in combination with reduced predation pressure and a spatial limitation of suitable habitat due to fragmentation cause a rapid increase of urban wildlife populations [5,10,11], and several studies suggest greater longevity of the individuals within these populations too [12,13,14]. On the other hand, density-dependent factors that limit population growth, such as the risk of disease and parasite transmission, as well as intraspecific competition, are likely to be higher in urban populations (reviewed by [15,16,17,18]). Therefore, urban populations within cities might suffer from higher intrinsic mortality rates compared to rural populations and/or are in less good health conditions [11,18,19]. Furthermore, the risk of traffic accidents can be increased in cities [12], also shown for European rabbits [20], and exposure to chemicals (in birds [21] and red foxes [22]) further negatively influences the health conditions of urban wildlife populations (see also [18,23,24]).
The spread of urban structures is one of the major causes of the global loss of biodiversity; however, cities nowadays also have the potential to serve as new habitats for wildlife [25,26]. While many studies prove that plant and animal species that were formerly assumed to be absent from cities are now thriving in urban areas, empirical data on the influence of urban landscape features on behavior, ecology, and physiology are yet only available for some species. A deeper understanding is highly necessary not only from a conservation point of view but also regarding potential threats that originate from urban wildlife populations, such as the transmission of diseases to other organisms, including humans.

1.2. Aim of This Study

The European rabbit Oryctolagus cuniculus (Linnaeus, 1758) is an excellent model organism to add knowledge to the question of how urban conditions affect the physiology and health status of a small herbivore urban mammal. Wild rabbits have been extensively studied under controlled field environments, and it has been found that harsh weather conditions and low food availability have a strong negative impact on the body condition of breeding females, as well as on the survival rates of yearlings [27,28,29]. Aside from the spread of introduced diseases such as myxomatosis since the 1950s (in Great Britain [30] and rabbit hemorrhagic disease (RHD) in the late 1980s in Spain [31]), especially intensified agricultural practices and altered forms of land use are major threats to rabbit populations all throughout rural areas of Europe [32,33,34]. While German rural populations also locally undergo severe declines, German city authorities aim to control high rabbit densities within urban areas through the application of a yearly hunting regime in the past (e.g., Frankfurt am Main, further Frankfurt). However, no information on the health status and body conditions of rural and urban European wild rabbits is available. Our study aims to fill this gap by comparing the physiology of urban and rural populations of O. cuniculus for the first time.
In earlier publications, we demonstrated that the here studied urban rabbit populations in and around Frankfurt reached higher densities (up to 25.0 individuals per ha) compared to rural populations (max. of 1.0 individuals per ha, see [35,36,37]). Moreover, urban rabbits build smaller rabbit burrows with fewer entrances and live in smaller social groups [36]. For the studied urban rabbits, we further calculated the smallest home ranges that have ever been reported for this species (95% MCP = 0.5 ha [38]). Through behavioral focus observations, we further found higher agonistic behavior and, thus, the evidence for higher intraspecific competition amongst urban rabbits compared to rural ones [36,39].

1.3. Hypotheses

We tested for two contradictory hypotheses: (1) Urban populations benefit from warmer temperatures, a higher, more continuous food source availability throughout the year, as well as from being less exposed to predation by natural predators compared to their rural conspecifics. This will lead to greater longevity and a better overall body condition, which will be reflected in an overall higher age, higher weights, healthier blood parameters, and a higher calorimetric stomach content. Furthermore, urban populations benefit from a perpetual grass-cutting regime that reduces the risk of infection with parasites through grazing. An overall healthier body condition will further favor fewer parasite infestations in both—the intestines and the feces of urban rabbits. In contrast, (2) because urban rabbits experience higher risks of disease transmission and intraspecific competition due to higher densities as well as face higher risks of intoxication and traffic accidents, their longevity is reduced, and they show clear signs of poorer body conditions compared to the rural populations. This will also be reflected in higher intestinal parasitization levels, as well as higher parasite loads in the feces of urban rabbits. Moreover, the parasite diversity of feces from urban rabbits is expected to be greater as a warmer microclimate in the city favors the reproduction of many parasites, whereas only a few can persist and reproduce under cooler conditions.

2. Materials and Methods

2.1. The Ethical Statement

For our present study, only wild rabbits had been used that were killed within the framework of the yearly hunting season performed by professional local hunters. Some of these hunters are also hired by the city of Frankfurt in order to control rabbit populations using ferrets between October and March (hunting license ID 1000250221). This annual rabbit hunting in and around Frankfurt is not related to our research and would have taken place regardless. Therefore, no rabbits have been purposely killed for this study. We merely took advantage of the hunting season by attending the local hunters and purchasing the rabbit carcasses for our research. Our study on European rabbits was further approved by the Animal Welfare Commission of the State of Hesse (ID: V54-19c 20/15–F 104/59 issued 08/04/2011).

2.2. Selection of Study Sites

For the analysis of the rabbit carcasses, we included n = 34 individuals stemming from 4 different rural areas around Frankfurt (Germany) and n = 39 animals from 5 different urban sites within the city center of Frankfurt (see Figure 1). Concerning the fecal samples, we selected 8 green urban areas (measuring between 1 and 4.9 ha in size) in the city center of Frankfurt, 4 parks at the periphery of the city, henceforth referred to as “suburban” (between 5.5 and 30.2 ha) and 3 nearby rural study sites (all 36 ha; Figure 1).
In the case of the urban and suburban study sites, short-cut meadows were the dominant landscape element, with a grass-cutting regime of up to once a week from March till November by the Frankfurt Green area Management “Grünflächenamt”. The dimensions of our study sites were clearly defined by park borders like streets or pathways. In the rural areas, open landscapes were dominated by agriculturally used areas in which low-grass orchard meadows had a sheep grazing regime of two to three times per year. Rape and wheat fields alternated, and between the meadows and fields, only a few patches of denser vegetation were present—mainly comprising blackberry bushes. Rabbit densities for some of the study sites have been assessed in previous studies [35].

2.3. Standard Blood Parameters

Rabbits were caught using domestic ferrets (Mustela putorius furo), which flushed rabbits out of their burrows. At urban study sites, cages were placed in front of the burrows, and rabbits were professionally killed by professional hunters after they got trapped in the cage. At rural study sites, animals were mostly shot by the hunters from afar as soon as the rabbits were flushed out of the burrows by ferrets. This was due to the fact that it was impossible to cover all the burrow entrances at rural sites because there were too many of them belonging to one burrow system (see also [36]).
Immediately after death, we used heparinized syringes to take blood samples from the cranial vein and quantified the glucose level directly in the field using a portable glucose meter (Omnitest 3, B. Braun Melsungen AG, Melsungen, Germany). Individuals were then weighed and sexed on site, and all carcasses, as well as the blood samples, were transported on ice to our laboratory at the Goethe University of Frankfurt. While carcasses were stored at −20 °C for later examination, blood samples were immediately prepared for a complete examination of standard blood parameters.
For a total of 70 blood samples, the complete blood picture including the mean corpuscular volume (MCV), mean corpuscular hemoglobin concentration (MCHC), and red blood cell counts (RBCs)—in addition to the aforementioned parameters—were assessed by following the manual provided in [40].

2.4. Body Size and Organ Weights

Prior to dissection, each rabbit was defrosted at room temperature. We measured the total body length from the snout to the basis of the tail to the nearest centimeter [41]. We checked for external signs of injuries and inspected ears, coat, skin, nostrils, and perianal regions for ectoparasites such as lice, ticks, and fleas. Ectoparasites were extracted using fine forceps and were counted but not further specified. In the case of lice and fleas, we categorized the infestation into 4 groups. We based our categories on the size of the area of the rabbit’s body that had been infested (group 0: no infestation, group 1: low infestation, group 2: medium infestation, group 3: high infestation, group 4: extreme high infestation).
We then opened the body cavity by a ventral cut from the pelvis to the sternum and fixated both sites of the body in order to remove the alimentary tracts, liver, and spleen for further examination of parasitization. Kidneys and adrenal glands were also removed from the carcass. Opening the diaphragm, heart, and lungs were removed from the thoracic cavity, cutting blood vessels and trachea. Finally, the brain was separated from the brain case. In total, we dissected 28 males and 44 females. The latter were checked for pregnancy.
All organs were separated from the surrounding fat tissue and placed in Petri dishes on ice containing physiological saline solution. The weights of abdominal organs, lungs, and heart were recorded with a digital scale (0.1 mg digits, ME204TE/00, Mettler Toledo, Giessen, Germany). We further screened organs for signs of any endoparasitization or illnesses under a dissection stereo microscope (OZP-15, Kern, Munich, Germany). A rabbit was classified as having myxomatosis if it had typical sores around its eyes, nose, base of ears, reproductive or excretory orifices, as well as having a general poor condition with a lower body weight on average.
Lastly, both eye lenses were removed, dried, and weighed in order to determine the individual’s age. We used an equation that allows determining the age of a rabbit in days from its eye lens weight [42].

2.5. Parasite Load of the Alimentary Tract

We screened organs of the alimentary tract for signs of endoparasites or illnesses under a dissection stereo microscope (OZP-15, Kern, Munich, Germany). The alimentary tract was separated into three regions: stomach, small intestine, and large intestine. The contents of each region were sieved through a 100 mesh (125 mm) sieve. The residues were collected and either examined fresh within 24 h or occasionally stored in 5% formalin (2% formaldehyde). Endoparasites were isolated with fine forceps, fixed in 4% borax-buffered formalin, and preserved in 70% ethanol with 5% glycerin. All cestodes were counted. According to the study of Frank et al., 2013 only one species (Cittotaenia denticulata) has been found in wild rabbits from that area [43]. In the case of the nematodes Trichostrongylus retortaeformis and Graphidium strigosum it was only noted whether these species were present because it was impossible to individually count them.

2.6. Caloric Measurements of Stomach Contents

We investigated potential links between standard blood parameters, organ gross anatomy, parasite patterns, and food quality by conducting caloric measurements of the stomach contents of all samples. For this, we removed the stomach content from the surrounding tissue, weighed all contents, and screened for the red stomach worm Graphidium strigosum (Nematoda, Trichostrongylidae). Afterwards, the stomach content was oven-dried at 60 °C for 72 h and re-weighted using a digital scale (0.1 mg digits, ME204TE/00, Mettler Toledo, Giessen, Germany). We stirred the ground stomach content and took three subsamples to measure the caloric content using a C200 oxygen bomb calorimeter (IKA-Werke GmbH & Co. KG, Staufen, Germany). Results are given as the mean value of these 3 measurements as the caloric value in joule/gram stomach content.

2.7. Collection of Feces Samples

Rabbits are exposed to various parasitic infections during their lifetime and can act as intermediate or final hosts for these infections. The reproductive cycle of many parasites includes a reproductive state such as eggs or oocytes that are well-equipped to survive even hard climatic conditions outside the host. In the case of the European rabbit, these eggs and oocytes can easily be detected in the rabbit feces.
Rabbits drop their feces accumulated into so-called “latrines”. A latrine was considered to be an accumulation of 20 or more pellets within an area of 20 × 30 cm2 [44]. Latrines close to the burrow are used by all members of the rabbit group for intra-group communication; latrines at the territorial borders are only used by dominant males [37,45]. We, therefore, only sampled latrines that were close to the burrow systems in order to collect feces from the entire rabbit groups.
In total, we collected 15 samples within each study site from at least 10 different latrines that belong to different rabbit burrows (see Figure 1). One sample consisted of at least 4 single fecal droppings from one single accumulation within one latrine (see also [45]). Therefore, it can be assumed that one sample belonged to only one individual, as rabbits drop more than one fecal pellet. However, since the goal of this approach was to get a general impression of the parasite load of rabbit feces, we did not further attempt to individually identify the samples. Therefore, we cannot exclude that several samples stem from the same individual. After collecting, samples were put in 2 mL Eppendorf tubes and stored at −18 °C until analysis.
European rabbits usually leave their burrows during the night to use their latrines [36,37]. Therefore, rabbit feces were sampled during the first week of September, October, and November 2011, shortly after sunrise, to ensure that only fresh samples were considered for this study. We collected only large, freshly dropped fecal pellets in order to exclude samples from juveniles who generally have a higher parasite load [46].
All study sites were sampled simultaneously within a maximum of 3 days in between sampling. We further resampled the urban study sites and two rural study sites (Bad Vilbel and Kriftel) in February, March, and April 2012. Due to changes in rabbit density and harsh weather conditions, no samples could be collected for Miquelanlage in October and Dreieich Götzenhain in September 2011 (see also Supplementary Material).

2.8. Parasite Load of Feces

We defrosted the samples, weighed (mean sample weight between 1 and 3 g), and diluted the pellets in a 100 mL beaker filled with 30 mL flotation solution (Coprosol, Albrecht GmbH & Co. KG, Lindlar, Germany specific density = 1.270). The dilution was then filtered through a mesh of 0.63 mm pore size into a 200 mL beaker. This beaker was then further filled with a flotation solution up to 60 mL in order to flush remains through the mesh into the final dilution. This dilution was mixed, and two samples were transferred into a modified McMaster counting chamber with two chambers. In order to allow oocytes and helminth eggs to float to the surface, we waited 10 min before counting the number of eggs per gram of feces (EpG) and oocytes per gram of feces (OpG), respectively, using a microscope with 100 (Objective 10×, Ocular 10×).
OpG/EpG was calculated using the following equation:
O p G / E p G = n u m b e r   o f   o o c y t e s   i n   2   c o u n t i n g   c h a m b e r s N × v o l u m e   o f   s u s p e n s i o n   l i q u i d ( m L ) a m o u n t   o f   u s e d   f e c e s g × s i z e   o f   c o u n t i n g   f i e l d c m 2 × h e i g h t   o f   c o u n t i n g   c h a m b e r c m × n u m b e r   o f   c o u n t i n g   c h a m b e r s
  • Volume of dilution = 60 mL Sodium nitrate;
  • Size counting area = 1 cm2;
  • Height of the counting chamber = 0.15 cm;
  • Number of chambers = 2.
The lowest level of detection for parasite states with this method is a value of 50 EpG and 50 OpG, respectively. Infestations with coccidia (Eimeria) were quantified by the occurrence of coccidia oocytes per gram of feces. For a more detailed determination of the different Eimeria species, we filled half of a plastic bin (Fecal Ova 3 StepTM, Kruuse, Langeskov, Denmark) with the fecal pellet dilution. We then filled up the bin with more dilution again using the according mesh for this sample until the dilution formed a convex surface on the bin. A cover slip was placed for 20 min on the surface of the solution, and the floated oocytes attached to the cover slip were examined under a microscope with 100× magnification. We counted 100 oocytes and classified them into oocytes from 8 different Eimeria species known to be present in the intestines of the European rabbit. For classification, we followed the descriptions of [47,48].

2.9. Statistics

All statistical analyses were conducted in R version 4.4.2. We used the following packages: tidyverse (2.0.0), rstatix (0.7.2), readxl (1.4.3), ade4 (1.7–23), psych (2.4.12), vegan (2.6–10) and MASS (7.3–61). Since we were not able to assess some variables from caught individuals, the sample size varies slightly for the different analyses.

2.9.1. Sex, Age, and Body Weight

We tested for differences in the distribution of males and females between urban and rural rabbits using a chi-square test. We further tested for differences in age and body weight using two different ANOVAs. In ANOVA 1, we tested whether urbanity, sex, season, and/or age had an influence on the rabbits’ body weight. In ANOVA 2, age was the dependent variable, and urbanity and season were the explaining variables.
Age and season were divided into categories. Age: group 1 = rabbits ≤ 1 year, group 2 = rabbits > 1 year; season: autumn (November, December) and winter (January, February, March).

2.9.2. Standard Blood Parameters

In order to test for differences in blood parameters between rural and urban rabbits, we first used Bartlett’s test of Sphericity to test the hypothesis of no relation between variables and, thus, whether a correspondence analysis is applicable. The p-value of Bartlett’s test of Sphericity was highly significant (p = 1.0349 × 10⁻¹⁷), but the Kaiser–Meyer–Olkin (KMO) test indicated that this data set is not suitable for a PCA. We, therefore, used all blood parameters (previously tested for normal distribution, BoxCox transformed, if necessary, all z-score standardized) in a multivariate analysis of covariance (MANCOVA). Predictor variables for the MANCOVA included urbanity, season, and age as a numerical covariate (polynomial regression model). However, we were not able to confirm the normal distribution of the variables “% of granulocytes” and “% of monocytes” because of too many “0” values. We, therefore, decided to exclude these variables from the analysis.

2.9.3. Body Length and Organ Gross Anatomy

The p-value of Bartlett’s test of Sphericity was highly significant (p = 3.175 × 10−70), and the overall MSA of 0.75 indicated a good approach for a PCA. The variable “spleen” had a low MSA of 0.2 and was therefore not included in the PCA. The variable “thymus” had too many missing values and could also not be considered for the analysis.
To test for the degree of discrimination between urban and rural sites considering organ weights, a between-class analysis (BCA) using the following classes: rural = 0 and urban = 1 was used. The significance of the explained variance was tested against simulated values obtained after 10,000 permutations of the rows of the trait composition arrays (Monte-Carlo test).
In addition, we calculated the percentage of relative organ weight compared to the body weight and used these values (previously tested for normal distribution, BoxCox transformed, if necessary, all z-core standardized) as well as the body length and the energy content of the stomach as dependent variables in a MANCOVA (see above). The explaining variables were urbanity and season. Age was used as a numerical covariate.
For our analysis, we only included the blood and organ data of rabbits with less than 16 missing values.

2.9.4. Parasite Prevalence, Mean Intensity, and Mean Abundance in Dissected Rabbits

The prevalence for all found parasites in urban and rural rabbits’ carcasses was calculated according to [49]. Rabbits were considered infected with the respective ecto- and endoparasite taxon if at least one specimen was obtained from the carcass and differentiated as such. The intensity of infection (that is, the number of parasites of a nominated taxon obtained from an infected rabbit) and the abundance of parasites (defined as the number of conspecific parasites living in or on all rabbits in the same population) were measured for all ectoparasites as well as the endoparasites Passalurus ambiguus (nematode) and Cittotaenia denticulata (cestode). Moreover, we investigated individual parasite loads of Passalurus ambiguus and Cittotaenia denticulata between urban and rural rabbits by calculating an individual parasite index (IPI) following [49].
I P I = i = 0 i = n p 10 × s m i 1 × n i × s t i 1
  • ni = individual number of parasite species i;
  • np = number of parasites entering the index;
  • sti = Standard deviation (SD) of parasite I in all rabbits present in the data set;
  • smi = maximum of the term n i × s t i 1 for parasite species i.
Since the data were not normally distributed, and we were not able to transform them, we used non-parametric Kruskal–Wallis as well as Dunn’s pairwise comparison tests to check for differences between urbanities. To assess the strength of group differences in the Kruskal–Wallis tests, we calculated effect sizes using the epsilon-squared (ε2) statistic.

2.9.5. Parasite Prevalence, Mean Intensity, and Mean Abundance in Rabbit Latrines

We used the same approach as described above. First, we asked whether the feces from European rabbits from the rural, suburban, and urban areas differed in their IPI. Second, we asked whether the diversity of parasites within the rabbit feces varied among sites. For this reason, we calculated the Shannon–Wiener diversity index (H) [50]. Since the data were not normally distributed (Shapiro–Wilk normality test for IPI: W = 0.59847, p-value < 2.2 × 10⁻¹⁶; for H: W = 0.75535, p-value < 2.2 × 10⁻¹⁶) and we were not able to transform them, we used non-parametric Kruskal–Wallis as well as Dunn’s pairwise comparison tests to check for differences between urbanities as well as months. In order to control for the increased risk of Type-I errors when conducting multiple comparisons, we adjusted the alpha levels by using the Bonferroni correction.

3. Results

3.1. Sex, Age, and Body Weight

A chi-square test of independence was performed to examine the relationship between urbanity and sex of the caught rabbits. We found no significant relation with a chi-square of χ2 (1, n = 74) = 0.752, p = 0.3858. However, the relation between the variables “season” and “sex” of the caught rabbits was significant: χ2 (1, n = 74) = 4.912, p = 0.0267. More females had been caught during autumn (29 females and 12 males) compared to winter (14 females and 19 males). In total, we found three females to be pregnant, and all came from urban areas and had been caught in late winter.
The results of the two ANOVAs clearly showed that the factors “urbanity” and “age” had an impact on the body weight of the caught rabbits (F = 9.934, p = 0.03). Urban rabbits were significantly lighter (mean body weight in g ± standard deviation SD: 1508.80 ± 318.47 g) compared to rural rabbits (1643.59 ± 182.42 g). Rabbits ≤ one year old had a significantly higher body weight (1580.27 ± 272.91 g) compared to rabbits older than one year (1482.99 ± 286.97 g). Neither urbanity nor season had an effect.

3.2. Standard Blood Parameters

As shown in Table 1, all mean values for the assessed blood parameters for urban and rural rabbits were within healthy ranges for domestic rabbits, according to [51]—except for the percentage of pseudoeosinophile granulocytes and lymphocytes. The percentage of pseudoeosinophile granulocytes was lower in both urban and rural rabbits, whereas the percentage of lymphocytes was higher. Unfortunately, we were not able to account for the number of leukocytes and thrombocytes due to low blood quality.
The results of the MANCOVA revealed that the values for glucose (F = 5.240, p = 0.027), hematokrit (F = 18.479, p ≤ 0.001), hemoglobin (F = 7.178, p = 0.010), MCV (F = 4.229, p = 0.046), and % of pseudoeosinophils (F = 8.347, p = 0.006) were all significantly higher in urban rabbits compared to rural ones. The % of lymphocytes (F = 9.974, p = 0.029) was significantly lower in urban rabbits compared to rural ones.
The amount of hemoglobin was further influenced by season (F = 4.084, p = 0.049), being lower in autumn (mean hemoglobin in g/dL ± SD: 11.30 ± 2.46) and higher in winter (12.56 ± 1.58).

3.3. Body Length and Organ Weights

In Table 2, we provided the descriptive data for the body length, the organ weights relative to the body weight (in %), and the energy content of the stomach between urban and rural rabbits.
The correlation coefficients of organ traits of urban and rural European rabbits were moderate to high (determinant of correlation matrix = 0.000158). Thus, the data set is suitable for the reduction process. The PCA produced as many components as variables, which is expected. However, in line with the standard application of PCA for dimensionality reduction, we retained only the first six principal components that cumulatively explained 92% of the total variance ((PC1 = 24%, PC2 = 19%, PC4 = 15%, PC5 = 13%, PC3 = 12%, and PC6 = 8%). After extraction of the first six principal components, 14.55% of the residual correlation coefficients remained above the 0.05 threshold, suggesting that the retained components capture the major structure of the original correlation matrix.
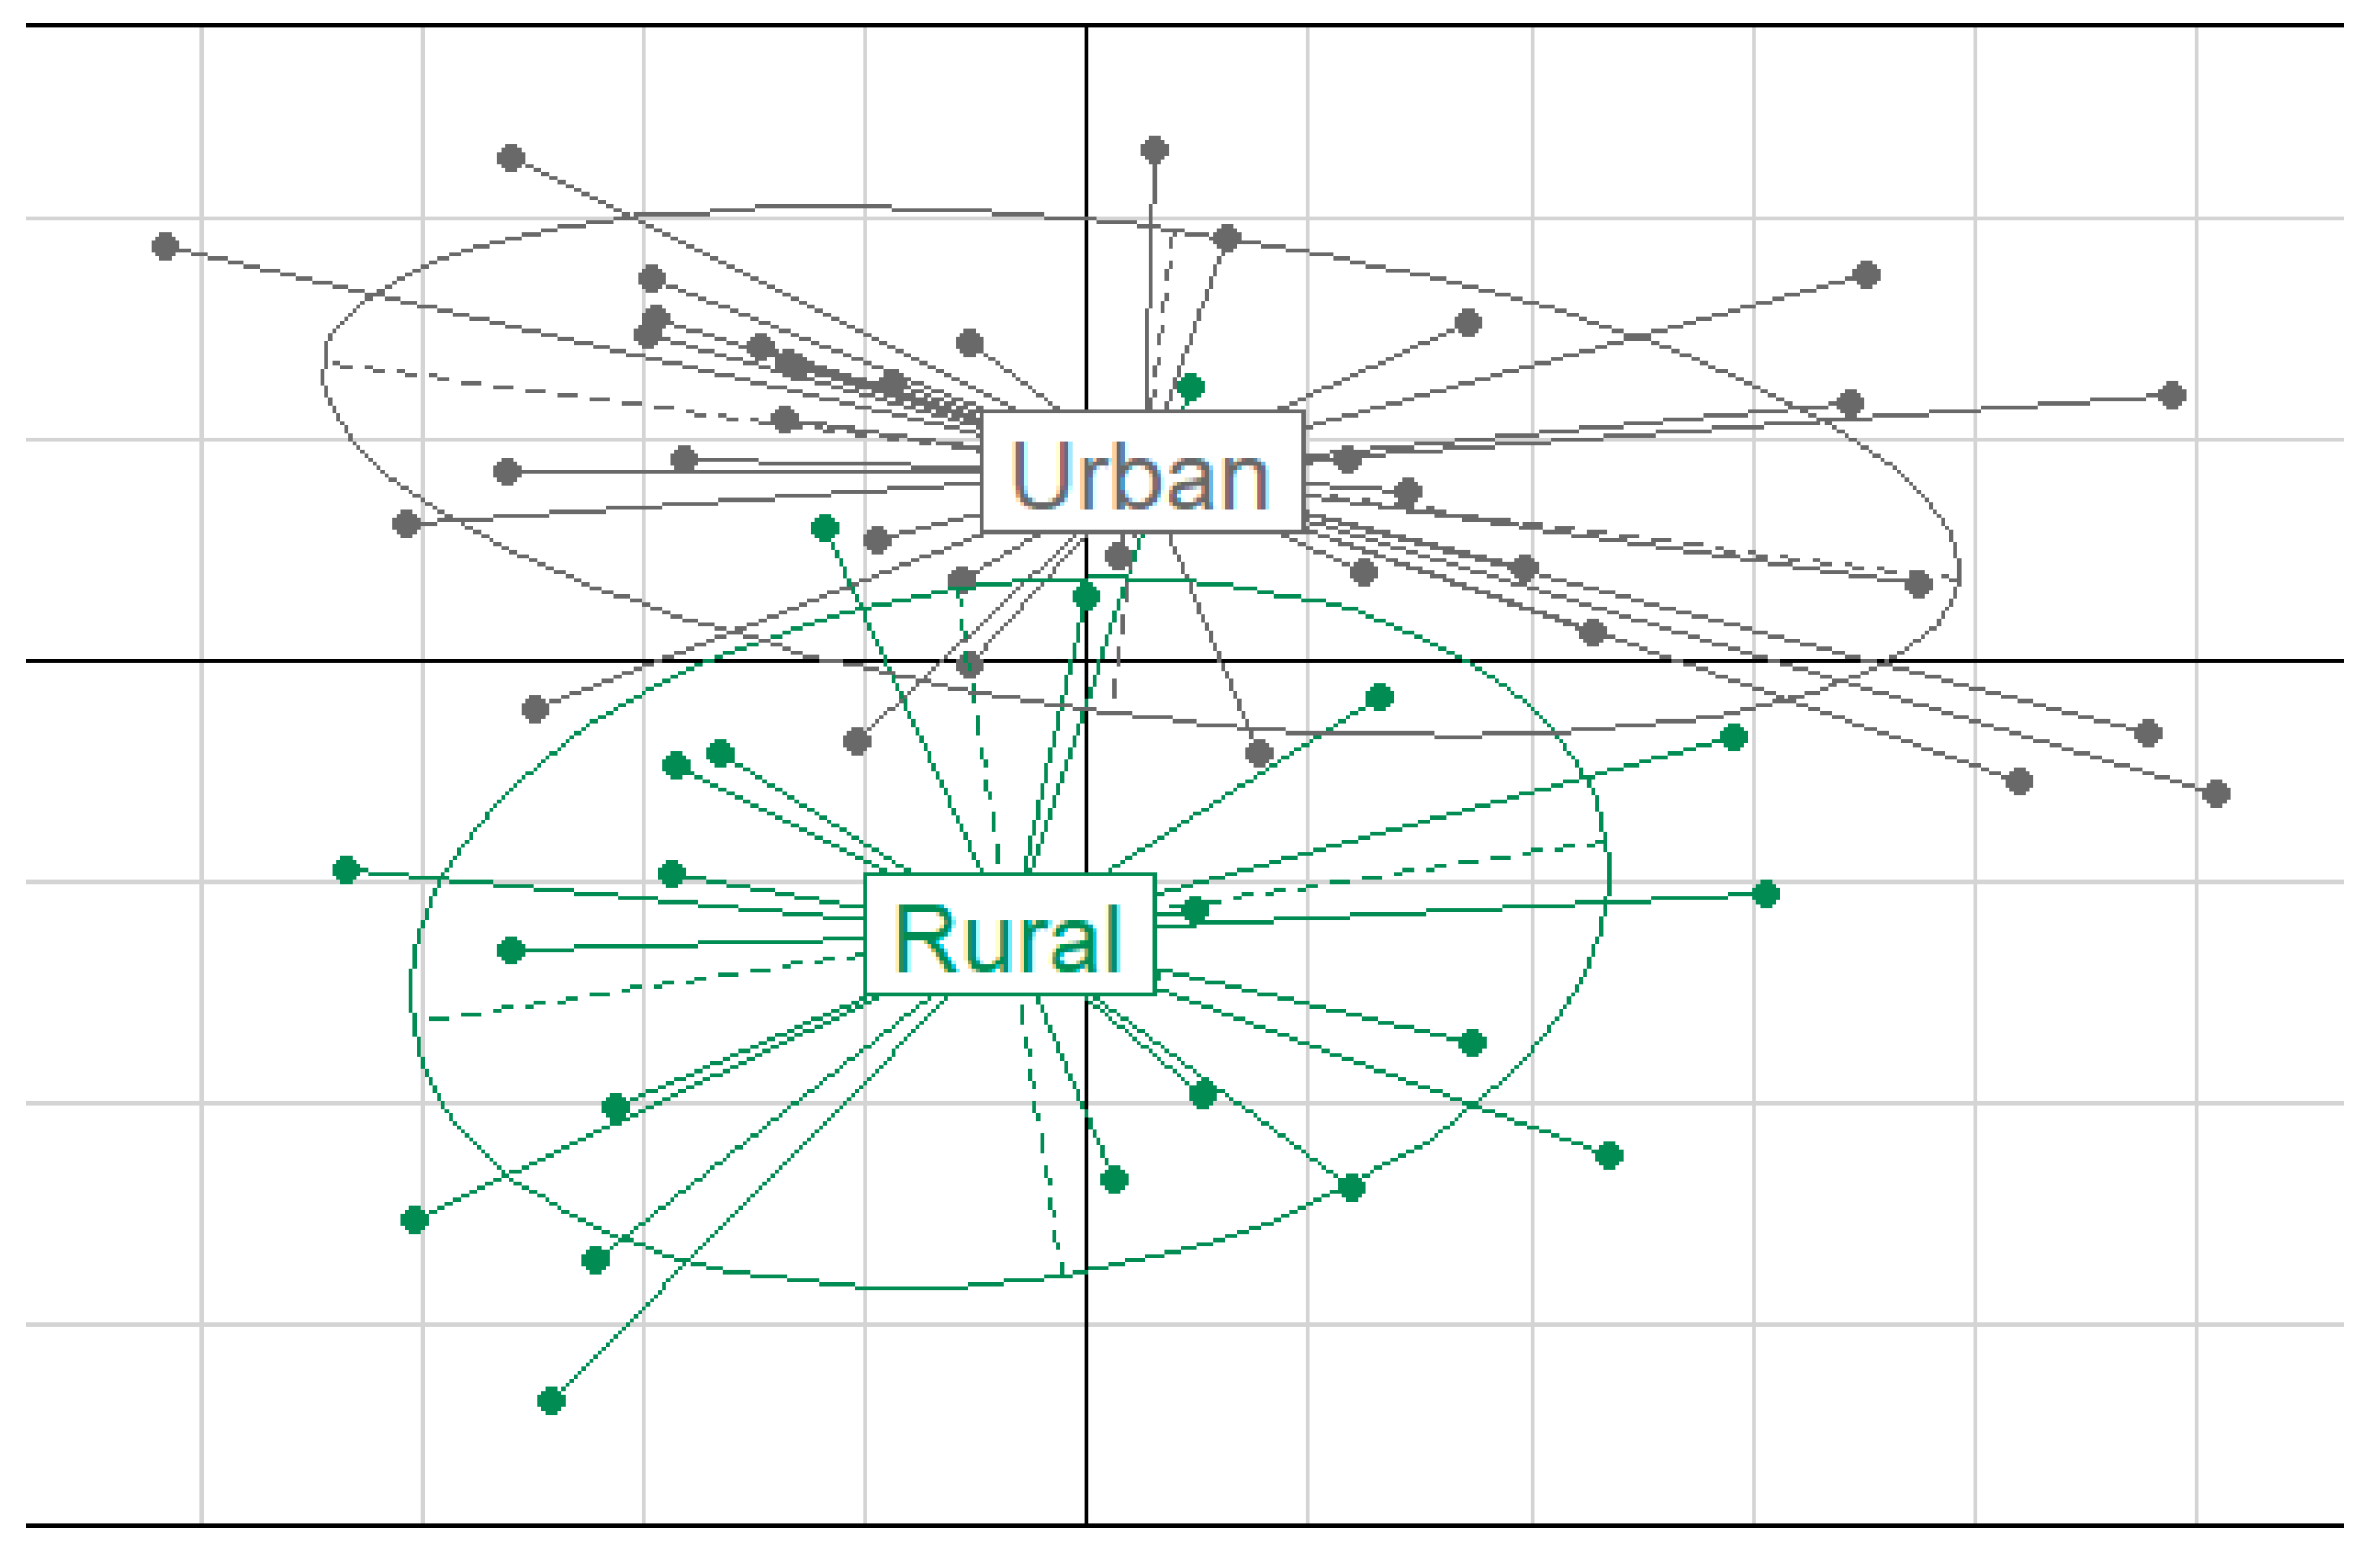
To test for differences in organ trait composition between urban and rural individuals, a BCA was performed using the retained PCA scores as input. The between-group variance explained by urbanity was 11.17% (Monte-Carlo permutation test with 10,000 perrmutations, p = 0.0003), indicating clear group separation in the trait space (Figure 2).
The influence of urbanity on the organ weights of rabbits was also confirmed by the results of the MANCOVA (F = 14.789, p ≤ 0.001). Furthermore, season (F = 8.350, p ≤ 0.001) as well as age (F = 2.327, p = 0.004) influenced the organ and body weights of rural and urban rabbits. The stomach (F = 29.485, p ≤ 0.001), intestines (F = 6.705, p = 0.013), liver (F = 22.309, p0.001), heart (F = 19.564, p ≤ 0.001), lung (F = 27.959, p ≤ 0.001), and brain (F = 5.052, p = 0.029) were significantly heavier in urban rabbits. In contrast, the right kidney (F = 6.299, p = 0.016), the left kidney (F = 5.675, p = 0.021), and the storage fat around the kidneys (F = 4.383, p = 0.042) were significantly heavier in rural rabbits. Rural rabbits also had a greater body length (F = 12.184, p = 0.001). The body length was further influenced by season (F = 15.848, p ≤ 0.00; see also Table 2). Rabbits caught during winter were smaller (body length in cm ± SD: 41.190 ± 2.97, n = 33) compared to the ones caught in autumn (44.36 ± 3.67, n = 41).
Please note that we had to exclude three individuals from the data set due to missing values (“U6”, stomach content was not measured; “R45” and “U2” age could not have been determined).

3.4. Parasites of the Dissected Rabbits

In Table 3, we listed an overview of the prevalence, mean intensity, and mean abundance of ecto- and endoparasites found on/in the dissected rabbits. For some parasites, we were only able to provide the prevalence as it was impossible to account for the exact number.
The Kruskal–Wallis and Dunn’s pairwise comparison test revealed a significant difference between the IPI (based on Passalurus ambiguus and Cittotaenia denticulata) of rural and urban rabbits (x2(1) = 5.91, p = 0.015, n = 71). The effect size was moderate, explaining 7.11% of the variance. Sex and season had no significant effect on the IPI. The infection with Passalurus ambiguus was significantly higher in rural rabbits compared to urban rabbits. In contrast, no rural rabbit was infected by Cittotaenia denticulata, while 15.79% of all examined urban rabbits were infected.

3.5. Feces Collection from Different Study Sites

In Table 4, we listed an overview of the prevalence, mean intensity, and mean abundance of endoparasite eggs and oocytes found in rabbit latrines in urban, suburban, and rural areas. For more detailed information, please see the Appendix A and Supplementary Material.

3.5.1. Parasite Index

The Kruskal–Wallis (x2(2) = 8.8, p = 0.012, n = 794) and Dunn’s pairwise comparison test p = 0.0132) revealed a significant difference between the IPI of rural and suburban rabbit populations (urban vs. rural: p = 0.0132; suburban vs. urban: p = 0.0132). The IPI was lowest in suburban rabbits (mean value for IPI ± SD: 1.0 ± 1.59), medium in urban rabbits (1.32 ± 2.10), and highest in rural ones (1.68 ± 2.80). However, the effect size was rather small (explaining 0.86% of variance).
A Kruskal–Wallis (x2(5) = 35.86, p ≤ 0.001, n = 794) and Dunn’s pairwise comparison test (p ≤ 0.0225) also revealed a significant difference between the IPI of the month of November compared to all other sampling months (effect size = 0.0392). In November, the IPI was the lowest.

3.5.2. Shannon–Wiener Index

Another Kruskal–Wallis and Dunn’s pairwise comparison test confirmed a significant difference in the Shannon–Wiener Index of the parasite communities within the feces of rural populations compared to the suburban and urban rabbit populations (effect size = 0.0189, Figure 3). In the rural areas, the parasite diversity within the rabbit latrines was significantly higher.
The season further influenced the parasite communities in rabbit latrines. The Shannon–Wiener index of March and April was significantly higher compared to the ones from September, October, and November (p values of Dunn’s pairwise comparison test with Bonferroni correction were all p ≤ 0.001). Additionally, the parasite community in February was significantly higher compared to November (p = 0.01).

4. Discussion

In our study, the body condition, blood parameters, parasite load, and stomach calorimetry of European rabbits were compared between rural and urban environments. The results of our study revealed significant differences in body weight, organ weight, parasitization, and blood parameters among environments.

4.1. Rabbit Body Condition and Parasitization Is Associated with Habitat Type

Concerning our initial hypotheses, some results point towards the acceptance of hypothesis 1 and some to hypothesis 2. While we found no differences in the age structure, rural rabbits had an overall heavier body weight compared to their urban conspecifics. This can mainly be explained by the fact that rural rabbits also have an average longer body length of 2.99 cm and significantly more fat tissue around their kidneys. Although urban rabbits had a lower body weight, some of their organs, such as the liver, the stomach, the lung, the intestines, and the brain, were significantly heavier. Along with these results, we found further significant differences in the blood measurements.
Overall, all measured blood parameters of the rural and urban rabbits were within ranges documented for healthy domestic rabbits, except the percentage of lymphocytes and pseudoeosinophile granulocytes. The first was higher and the second was lower in both urban and rural rabbits. In general, rabbits that cope with an infectious disease do not typically have a higher white blood cell count but rather show a shift from lymphocyte-predominant to neutrophil-predominant differential counts. This was not the case in our study. Urban rabbits had significantly higher values in hemoglobin and hematocrit as well as a higher percentage of monocytes, basophils, and pseudoeosinophils. The mean corpuscular volume, which represents the average size of the red blood cells, was also higher in urban rabbits compared to rural ones. From a veterinarian’s point of view, these could all be early signs of chronic heart insufficiencies and illnesses of the lung. Moreover, the fact that the hematocrit content was higher in urban rabbits could be a sign of dehydration [51]. This theory finds support by the fact that we found several urban rabbits to have remarkably dry skin. Moreover, all rabbits that showed signs of illnesses, such as myxomatosis or coccidiosis, were caught in urban study sites. In accordance with other studies, urban females started earlier with reproduction compared to rural ones. While we found three females being pregnant in late winter, we found none from the rural area.
The examination of parasitation in rural and urban carcasses further revealed that rural rabbits were much more often infested by high numbers of the parasites P. ambiguous, T. retortaeformis, and G. strigosum. The mean intensity of P. ambiguous was 2.25-fold higher in rural rabbits compared to urban ones. Rural rabbits were also more often hosts for fleas, while in urban rabbits, mites were more often present. The most striking difference concerning the parasitization was the fact that the prevalence of C. denticulata was 0% in rural rabbits but 15.79% in urban rabbits. Severe infestations with nematodes and cestodes cause catarrhal inflammation of the small intestine, leading to diarrhea, emaciation, and sometimes even death. We found evidence of intestinal inflammation in all urban rabbits that were infected by C. denticulata. In these cases, the parasite numbers seem to have been high enough to visibly affect the rabbits’ body parameters.
These results were partly congruent with the analysis of the amount of parasite eggs and oocytes in the feces of urban, suburban, and rural rabbit latrines. At rural study sites, rabbit latrines had a higher mean parasite index and were also infested by a larger range of parasite species. Here, we found significantly more eggs of the nematode P. ambiguous, also at a much higher intensity. As expected, we found the highest prevalence caused by oocytes of the single-cell organism Eimeria sp. A prevalence between 92–96% occurred in all three habitats: urban, suburban, and rural. The nematode G. strigosum had the highest prevalence in urban latrines, with 35.53%, whereas the prevalence of this parasite was comparable between rural and suburban latrines. The mean intensity of the eggs of C. denticulata in rabbit latrines was comparable between sites, but the prevalence was significantly higher in rural latrines. This comes as a surprise since we found no adult individuals of C. denticulata in rural rabbit carcasses. Now, how can all these differences in body weight, organ weight, blood parameters, and parasite load be explained, and what do they mean in terms of future rabbit population dynamics?

4.2. Different Lifestyles in Urban and Rural Rabbits

Since we found no differences in the age or sex distribution among the rural and urban rabbits, we assume that differences in the habitat quality are likely to influence the health and body conditions of wild rabbits. From previous studies on the here presented rabbit populations, we know that along the rural-to-urban gradient, rabbit and burrow densities increase [36]. These higher population densities were mainly explained by better habitat qualities such as access to food and shelter for burrow construction, warmer temperatures in the city, and lower predation pressure. In urban areas, the mosaic-like habitat is more heterogenic. Here, different habitat types such as green areas, gardens, wastelands, or railroads are changing on a small local scale. This habitat heterogeneity makes it easier for rabbits to find suitable areas for their burrow constructions and have food close by at the same time. In the studied rural areas, we mainly found burrows to be accumulated in the few small patches of denser vegetation that consisted of thick blackberry bushes. Rape and wheat fields, as well as orchard meadows and private gardens, surrounded the rabbit burrows (see also [36]).
The examination of standard blood parameters is a suitable approach to assess the overall health condition (e.g., signs of inflammations or occurrence of specific diseases in different populations [52]). Moreover, ref. [52] Tousson et al. (2011) found that parameters such as hemoglobin (Hb) and hematocrit contents (HCT), mean corpuscular hemoglobin (MCH), and white blood cell counts (WBCs) also relate to the quality of food individuals had access to. Especially the count of lymphocytes reflects the nutritional status since an abnormal rise in lymphocytes may be a result of malnutrition, among other factors [53]. Also, the amount of hematocrit was related to the type of diet. Interestingly, we found an abnormal rise in lymphocyte percentages in rural and urban rabbits. One could argue that together with the lower body weight and smaller body sizes, the higher numbers of lymphocytes are an early sign of malnutrition in urban rabbits. We argue that the competition for food is much higher in the denser populated urban areas—especially for young rabbits during the summer time. This idea would also be supported by the fact that rural rabbits had significantly more fat tissue around their kidneys compared to urban ones. In rural areas, rabbits have access to high-caloric food sources such as vineyards, canola or sugar beets, especially during summer and autumn.
According to [54], there are different maintenance levels for rabbits of different ages and reproductive states. However, in general, laboratory tests showed that domestic rabbits need approximately 450 kJ day−1 kg−1 [55,56]. In comparison, rural rabbits had a mean energy content of 17.93 kJ in their stomachs. At an average weight of 1.64 kg they would need 739.35 kJ per day. For urban rabbits, it would be 678.6 kJ per day due to the overall lower body weights. Our analysis of the energy content of the stomach showed no significant differences between urban and rural rabbits, but only season having an effect (on average 214 joules/g more in autumn). This suggests that the food quality was comparable between rural and urban areas. However, our analysis was merely a small snapshot of the rabbit’s diets and only focused on the energy content in the stomach. Several studies show that the dietary composition of rabbits is variable across seasons [54]. As we found grapeseed in the stomachs of rural animals but none in urban stomachs, one could assume that the diet of the rural rabbits is more diverse, also including seasonal fruits. However, we do know from personal observation that rabbits in urban areas are fed carrots, apples, and salads on a regular basis by pedestrians. An overall higher intake of food could also explain why the weight of the intestines in urban rabbits was much higher. Interestingly, we detected little gravel stones in the intestines of the urban rabbits, suggesting that while taking in their food, they also picked up pebbles. That could have been the reason why their stomachs were significantly heavier.
Previous research on the studied rabbit populations showed that the animals were most active in the early morning (≤4 h after sunrise), decreased activity around noon (>4 h and ≤10 h after sunrise), and spent increasingly more time outside their burrows starting again in the late afternoon (>10 h after sunrise, [39]). However, suburban and urban populations were more active above ground around noon and in the afternoon compared to their rural conspecifics. Instead of investing in anti-predator behaviors, suburban and urban rabbits spend more time grazing, moving around, and resting above ground. Although we did not quantify actual predation risk, we argue that urban populations are likely to experience less predation pressure by natural predators compared to rural sites [57]). This higher activity level of urban rabbits outside their protective burrow systems could also be an explanation for their heavier cardiovascular system. Regarding brain capacity in rodents, several studies show contradictory results, with both an increase and a decrease in brain capacity in urban areas [58]. Ref. [58] suggests that the predictability of urban habitats may be the cause of a decrease in brain capacity over time in urban habitats.
Another reason for the different organ weights in urban rabbits could be a higher degree of inbreeding. However, our previous study on population genetics revealed that the observed heterozygosity was significantly higher in the studied urban populations. Furthermore, the inbreeding coefficients were also lower, most likely reflecting the small population sizes and possibly ongoing loss of genetic diversity in structurally impoverished rural areas [59]).

4.3. Higher Infection Risks Through Rural Rabbit Latrines

The differences in parasite infestations between rural and urban species observed in various studies appear to be strongly taxon-dependent [60]. For example, hedgehogs (Erinaceus roumaincus Barrett-Hamilton, 1900, and Erinaceus europaeus Linnaeus, 1758) show a very high infestation with ectoparasites in urban areas [61]. For flea infestation, a negative correlation was observed between environmental heterogeneity (i.e., urbanization), while the number of ticks per host, however, correlated positively with the degree of urbanization of the habitat [61]. In addition to the population density of the hosts, environmental conditions such as vegetation, climate, and soil composition also influence the abundance of various ectoparasite species.
According to previous research, wild rabbits are used as intermediate and/or final hosts by Digenea (8 species), Cestoda (14 species), Nematoda (43 species), Acarina (15 species), Diptera (8 species), Phthiraptera and Siphonaptera (7 species), and Pentastomida (1 species) [62,63,64,65,66]. Also, several protozoan parasites are commonly found in both wild and domesticated rabbits, such as Eimeria intestinalis (Sporozoa) [67], Eimeria coecicola [68], Sarcocystis cuniculi (Sporozoa) [68], and Trypanosoma nabiasi (Flagellata) [69]. Species such as the microsporidian Encephalitozoon cuniculi [70], Cryptosporidium cuniculus [71], as well as the Sporozoa Toxoplasma gondii [72] are known as human pathogenics.
In our study, we also find that the intensity, prevalence, and abundance of rabbit parasites are highly dependent on the type of parasite. While tapeworm species rely on intermediate hosts during their developmental cycle, such as moss mites, infection with nematode species occurs directly through the ingestion of infectious stages with food. Due to their free-living stages, the various nematode species are directly dependent on environmental climatic conditions [41]. According to [73], yearly and seasonal changes in parasite infestation and communities are mostly the result of variations in weather conditions that influence the infectious stages and the presence of intermediate hosts. The authors found a low degree of fluctuation in the aggregation of Passalurus ambiguous in wild rabbits. They explain these results by the fact that the infectious stage of this parasite is likely to be less susceptible to environmental variation.
Moreover, cecotrophy also increases the likelihood of reinfection and, thus, the intensity of nematode infestation in rabbits [73]. In the green areas of the urban and suburban study sites, the grass-cutting regime was significantly more frequent compared to rural areas. This could also have reduced the amount of parasite eggs rabbits are reinfecting themselves with while grazing. However, ref. [74] found that parasites with complex life cycles were less prevalent in urban carnivore and primate populations than in non-urban populations. Moreover, ref. [74] found no difference in urban and non-urban prevalence for parasites in rodent and marsupial hosts. This meta-analysis also found no differences in the prevalence of parasites with simple life cycles in any host taxa. There, ref. [74] argue that there might be a disruption of some parasite transmission cycles in the urban ecological community. A closer look at the rabbits infected with cestodes within the urban study area revealed that all of the infected animals came from the same study sites, “Oskar-von-Miller-Straße” and “Deutschherren Ufer”. Since moss mites are of central importance in the cestode development cycle [73], their local distribution is a factor that limits the occurrence of cestodes in rabbits [75]. One possible explanation for the locally limited occurrence of cestodes in the urban rabbit population could, therefore, be the abundance of moss mites. This could have been influenced by the possibly different microclimates in the urban area. Given the direct proximity to the Main River in both of the study areas (both are on the opposite sites of the river), higher air humidity can be assumed, among other things. A study by Ref. [76] Smith et al., 1999 found a small but significant effect of humidity on survival for Psoroptes cuniculi; a moss mite species that parasitizes the ears of rabbits. Their lifetime was greater at 75–85% humidity than at 55–65% [76].

5. Conclusions

The process of urbanization is rapidly ongoing on a global scale. However, the effects of this process on wildlife health are not well documented. European rabbits are one example of a small mammalian wildlife species that is capable of surviving in urbanized environments and is commonly a host for a variety of endo- and ectoparasites. Wild rabbits are known for being very resilient, which mainly has to do with their ability to adapt their nutrition (great variety of choice and high use), their strong immune system, and other factors related to genetics and behavior. From our study, we can conclude that urban and rural environments differently shape the health and physiology of European wild rabbits. While rural rabbits exhibit higher overall body mass and fat reserves, urban rabbits show increased internal organ weights and altered blood parameters, possibly reflecting physiological adaptations to urban stressors such as dehydration or chronic exposure to pollutants. Parasite prevalence and diversity were generally higher in rural rabbits, though specific parasites were more common in urban populations. These findings suggest that urban life imposes distinct challenges that do not uniformly improve or impair health but rather reshape the animals’ physiological profiles in complex ways. The results also underscore the importance of monitoring urban wildlife for potential zoonotic risks to humans.

Supplementary Materials

The following supporting information can be downloaded at: https://maddyfellmeth.com/downloads/?et_fb=1&PageSpeed=off.

Author Contributions

Conceptualization, M.F., D.B., M.-L.S., A.S., and M.W.; methodology, M.F., D.B., M.-L.S., A.S., M.W., M.-C.U., and B.S.; software, M.F., B.H., and B.S.; validation, M.F. and B.H.; formal analysis, M.F. and B.H.; investigation, M.F., D.B., M.-L.S., A.S., and M.W.; resources, B.S.; data curation, M.F. and B.H.; writing—original draft preparation, M.F. and A.M.; writing—review and editing, M.F., B.H., and A.M.; visualization, M.F. and B.H.; supervision, M.F. and B.S.; project administration, M.F. and B.S.; All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Informed Consent Statement

Not applicable.

Data Availability Statement

Raw and analyzed data can be accessed through: https://maddyfellmeth.com/downloads/?et_fb=1&PageSpeed=off (accessed on on 3 June 2025).

Acknowledgments

We thank all technicians and students of the former group of Streit and Prinzinger who helped with rabbit dissection, analysis of the blood samples as well as the stomach content. We further thank Martin Plath, Hannes Lerp, and Raphael Frank for their scientific input. We thank Axel Seidemann and Yvonne Bohr for assisting with the field work.

Conflicts of Interest

The authors declare no conflicts of interest.

Abbreviations

The following abbreviations are used in this manuscript:
Hbhemoglobin
HCThematocrit contents
MCHmean corpuscular hemoglobin
WBCwhite blood cell counts
MCVmean corpuscular volume
MCHCmean corpuscular hemoglobin concentration
RBCred blood cell counts
EpGeggs per gram of feces
OpGoocytes per gram of feces
IPIindividual parasite index

Appendix A

Table A1. Descriptive statistics on parasite load in feces of rural, urban, and suburban rabbits for September 2011. Summary statistics are given at the beginning of the table; the prevalence (P), mean intensity (mI), and mean abundance (mA) of all parasites found were calculated according to Ref. [48], Bush et al. (1997). Descriptive statistics for all other months are available in the supplementary material. In total, we found 12 different parasite species.
September 2011 KriftelBad VilbelGötzenhainOstparkRebstockparkElli-Lucht-ParkMiquelanlageCity Centre
# samples301501515151576
# unparasitized10No data 01015
# of parasites in population 1210collected109101112
Protozoa
Eimeria sp.P [%]93.33100-10093.33100.0093.3390.79
mI ± SD8113.87 ± 12,320.5530,682.23 ± 33,876.47-4064.94 ± 4065.996398.86 ± 5885.096934.11 ± 22,654.0810,794.74 ± 11,931.396668.39 ± 20,389.14
mA ± SD7572.94 ± 12,065.0330,682.23 ± 33,876.48-4064.94 ± 4065.995972.27 ± 5906.796934.11 ± 22,654.0810,075.09 ± 11,830.395966.45 ± 19,380.86
Eimeria IP [%]93.33100.00-10086.6773.3393.3381.58
mI ± SD1318.96 ± 2839.8012,755.45 ± 22,435.69 1563.95 ± 2594.221626.20 ± 2576.457330.63 ± 23,141.345611.79 ± 9071.902155.29 ± 10,453.64
mA ± SD1187.07 ± 2718.8612,755.45 ± 22,435.69-1563.95 ± 2594.221409.37 ± 2453.005375.80 ± 19,843.765237.67 ± 8861.171786.62 ± 9539.62
Eimeria IIP [%]30.0033.33-93.3393.3373.338056.58
mI ± SD381.34 ± 350.751863.77 ± 1863.77-701.66 ± 865.741520.50 ± 2605.87843.97 ± 1554.44915.00 ± 1087.60546.22 ± 815.01
mA ± SD114.40 ± 255.99621.26 ± 1376.28-654.88 ± 853.691419.13 ± 2541.58618.91 ± 1428.87732.00 ± 1035.82309.04 ± 668.02
Eimeria IIIP [%]70.0060.00-93.3393.3373.3386.6780.26
mI ± SD1855.75 ± 2711.129649.85 ± 15,023.88-867.83 ± 923.401324.19 ± 1450.54790.87 ± 1554.442042.31 ± 1566.952819.97 ± 6657.63
mA ± SD1299.03 ± 2411.895789.91 ± 12,366.33-809.97 ± 917.591235.91 ± 1438.98579.97 ± 1362.711770.00 ± 1618.952263.40 ± 6061.00
Eimeria IVP [%]13.330.00-0.000003.95
mI ± SD41.99 ± 30.380.00-0.0000069.64 ± 77.38
mA ± SD5.60 ± 17.500.00-0.000002.75 ± 18.60
Eimeria VP [%]83.3366.67-86.6793.3340.0080.0072.37
mI ± SD5266.94 ± 8973.9812,277.95 ± 17,455.03-387.08 ± 798.761278.62 ± 1398.39300.24 ± 334.271553.39 ± 1457.221609.26 ± 3638.0
mA ± SD4389.12 ± 8404.358185.30 ± 14,888.13-335.47 ± 751.941193.37 ± 1387.37120.10 ± 251.171242.71 ± 1442.951164.60 ± 3170.78
Eimeria VIP [%]40.0046.67-66.6720.00040.0036.84
mI ± SD234.74 ± 297.66667.07 ± 599.84-151.02 ± 115.9599.42 ± 72.220273.52 ± 228.89207.97 ± 317.42
mA ± SD93.90 ± 217.46311.30 ± 522.36-100.68 ± 118.6319.88 ± 49.390109.41 ± 194.8176.62 ± 215.57
Eimeria VIIP [%]73.3393.33-93.3393.3386.6786.6771.05
mI ± SD622.79 ± 893.103267.34 ± 4963.60-682.46 ± 993.61739.86 ± 856.84279.01 ± 267.521031.51 ± 1085.44525.8 ± 1534.4
mA ± SD456.71 ± 809.973049.52 ± 4856.88 636.97 ± 973.54690.53 ± 847.48241.81 ± 266.42893.98 ± 1068.46373.59 ± 1311.98
Eimeria VIIIP [%]56.6726.67-20.006.6720.0053.3326.32
mI ± SD1643.17 ± 1862.65467.97 ± 329.90-44.81 ± 31.5059.78 ± ----19.74 ± 15.60165.95 ± 193.8372.64 ± 64.28
mA ± SD931.13 ± 1612.47124.79 ± 263.07-8.96 ± 22.043.99 ± 15.443.95 ± 10.0888.51 ± 161.6419.12 ± 45.64
Helmintha
CestodesP [%]30,0046.67-0.00013.3333.332.63
mI ± SD250.26 ± 225.331708.64 ± 1898.77 0.000203.21 ± 278.27606.10 ± 673.41113.93 ± 50.28
mA ± SD75.08 ± 166.17797.36 ± 1524.4-0.00027.09 ± 103.17202.30 ± 465.873.00 ± 19.25
NematodesP [%]20,0046.67-40.0013.3313.336.6719.74
T. retortaeformismI ± SD454.08 ± 477.81529.02 ± 434.83-258.29 ± 245.35154.88 ± 40.6969.57 ± 5.51328.76 ± ---171.30 ± 113.90
mA ± SD90.82 ± 271.09246.87 ± 394.54-103.31 ± 196.6020.65 ± 55.579.28 ± 24.5221.92 ± 84.8933.81 ± 84.45
G. strigosumP [%]10.000-6.6713.336.6713.3315.79
mI ± SD509.30 ± 631.410-155.52 ± --307.15 ± 10.83171.78 ± ---134.68 ± 30.77210.6 ± 356.25
mA ± SD50.93 ± 227.260-10.37 ± 40.1640.95 ± 108.1111.45 ± 44.3517.96 ± 48.1033.25 ± 156.81
P. ambiguusP [%]6.6753.33-33.3306.6705.26
mI ± SD362.33 ± 274.521864.01 ± 3277.28-172.96 ± 198.440171.78 ± ---0229.97 ± 119.42
mA ± SD24.16 ± 105.11994.14 ± 2509.3-57.65 ± 134.73011.45 ± 44.35012.10 ± 56.94

References

  1. Contesse, P.; Hegglin, D.; Gloor, S.; Bontadina, F.; Deplazes, P. The Diet of Urban Foxes (Vulpes Vulpes) and the Availability of Anthropogenic Food in the City of Zurich, Switzerland. Mamm. Biol.-Z. für Säugetierkd. 2004, 69, 81–95. [Google Scholar] [CrossRef] [Scilit]
  2. Coogan, S.C.P.; Raubenheimer, D.; Zantis, S.P.; Machovsky-Capuska, G.E. Multidimensional Nutritional Ecology and Urban Birds. Ecosphere 2018, 9, e02177. [Google Scholar] [CrossRef] [Scilit]
  3. Sogliani, D.; Mori, E. “The Fox and the Cat”: Sometimes They Do Not Agree. Mamm. Biol. 2019, 95, 150–154. [Google Scholar] [CrossRef] [Scilit]
  4. Beckmann, J.P.; Berger, J. Using Black Bears to Test Ideal-Free Distribution Models Experimentally. J. Mammal. 2003, 84, 594–606. [Google Scholar] [CrossRef] [Scilit]
  5. Reher, S.; Dausmann, K.H.; Warnecke, L.; Turner, J.M. Food Availability Affects Habitat Use of Eurasian Red Squirrels (Sciurus vulgaris) in a Semi-Urban Environment. J. Mammal. 2016, 97, 1543–1554. [Google Scholar] [CrossRef] [Scilit]
  6. Kark, S.; Iwaniuk, A.; Schalimtzek, A.; Banker, E. Living in the City: Can Anyone Become an “urban Exploiter“? J. Biogeogr. 2007, 34, 638–651. [Google Scholar] [CrossRef] [Scilit]
  7. Møller, A.P. Flight Distance of Urban Birds, Predation, and Selection for Urban Life. Behav. Ecol. Sociobiol. 2008, 63, 63–75. [Google Scholar] [CrossRef] [Scilit]
  8. Minias, P.; Janiszewski, T. Territory Selection in the City: Can Birds Reliably Judge Territory Quality in a Novel Urban Environment? J. Zool. 2016, 300, 120–126. [Google Scholar] [CrossRef] [Scilit]
  9. Marín-Gómez, O.H.; Dáttilo, W.; Sosa-López, J.R.; Santiago-Alarcon, D.; MacGregor-Fors, I. Where Has the City Choir Gone? Loss of the Temporal Structure of Bird Dawn Choruses in Urban Areas. Landsc. Urban Plan. 2020, 194, 103665. [Google Scholar] [CrossRef] [Scilit]
  10. Prange, S.; Gehrt, S.D.; Wiggers, E.P. Demographic Factors Contributing to High Raccoon Densities in Urban Landscapes. J. Wildl. Manag. 2003, 67, 324–333. [Google Scholar] [CrossRef] [Scilit]
  11. Pickett, S.T.A.; Frantzeskaki, N.; Andersson, E.; Barau, A.S.; Childers, D.L.; Hoover, F.A.; Lugo, A.E.; McPhearson, T.; Nagendra, H.; Schepers, S.; et al. Shifting Forward: Urban Ecology in Perspective. Ambio 2024, 53, 890–897. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Luniak, M. Synurbanization—Adaptation of Animal Wildlife to Urban Development. In Proceedings of the 4th International Urban Wildlife Symposium, Tucson, AZ, USA, 1–5 May 1999; Shaw, W.W., Harris, L.K., Vandruff, L., Eds.; University of Arizona: Tucson, AZ, USA, 2004; pp. 50–55. [Google Scholar]
  13. Partecke, J.; Schwabl, I.; Gwinner, E.; Rhythms, B. Stress and the City: Urbanization and Its Effects on the Stress Physiology in European Blackbirds. Ecology 2006, 87, 1945–1952. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. McDonnell, M.J.; Pickett, S.T.A. Ecosystem Structure and Function along Urban-Rural Gradients: An Unexploited Opportunity for Ecology. Ecology 1990, 71, 1232–1237. [Google Scholar] [CrossRef] [Scilit]
  15. Ditchkoff, S.S.; Saalfeld, S.T.; Gibson, C.J. Animal Behavior in Urban Ecosystems: Modifications Due to Human-Induced Stress. Urban Ecosyst. 2006, 9, 5–12. [Google Scholar] [CrossRef] [Scilit]
  16. Hamer, S.A.; Lehrer, E.; Magle, S.B. Wild Birds as Sentinels for Multiple Zoonotic Pathogens Along an Urban to Rural Gradient in Greater Chicago, Illinois. Zoonoses Public Health 2012, 59, 355–364. [Google Scholar] [CrossRef] [Scilit]
  17. Riley, S.P.D.; Sauvajot, R.M.; Fuller, T.K.; York, E.C.; Kamradt, D.A.; Bromley, C.; Wayne, R.K. Effects of Urbanization and Habitat Fragmentation on Bobcats and Coyotes in Southern California. Conserv. Biol. 2003, 17, 566–576. [Google Scholar] [CrossRef] [Scilit]
  18. Riley, S.P.D.; Serieys, L.E.K.; Pollinger, J.P.; Sikich, J.A.; Dalbeck, L.; Wayne, R.K.; Ernest, H.B. Individual Behaviors Dominate the Dynamics of an Urban Mountain Lion Population Isolated by Roads. Curr. Biol. 2014, 24, 1989–1994. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Strasser, E.H.; Heath, J.A. Reproductive Failure of a Human-Tolerant Species, the American Kestrel, Is Associated with Stress and Human Disturbance. J. Appl. Ecol. 2013, 50, 912–919. [Google Scholar] [CrossRef] [Scilit]
  20. Planillo, A.; Malo, J.E. Motorway Verges: Paradise for Prey Species? A Case Study with the European Rabbit. Mamm. Biol.-Z. Für Säugetierkd. 2013, 78, 187–192. [Google Scholar] [CrossRef] [Scilit]
  21. Getz, L.L.; Best, L.B.; Prather, M. Lead in Urban and Rural Song Birds. Environ. Pollut. 1977, 12, 235–238. [Google Scholar] [CrossRef] [Scilit]
  22. Dip, R.; Hegglin, D.; Deplazes, P.; Dafflon, O.; Koch, H.; Naegeli, H. Age- and Sex-Dependent Distribution of Persistent Organochlorine Pollutants in Urban Foxes. Environ. Health Perspect. 2003, 111, 1608–1612. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Forman, R.T.T.; Alexander, L.E. Roads and Their Major Ecological Effects. Annu. Rev. Ecol. Syst. 1998, 29, 207–231. [Google Scholar] [CrossRef] [Scilit]
  24. Etter, D.R.; Hollis, K.M.; van Deelen, T.R.; Ludwig, D.R.; Chelsvig, J.E.; Anchor, C.L.; Warner, R.E. Survival and Movements of White-Tailed Deer in Suburban Chicago, Illinois. J. Wildl. Manag. 2002, 66, 500–510. [Google Scholar] [CrossRef] [Scilit]
  25. Møller, A.P.; Díaz, M. Avian Preference for Close Proximity to Human Habitation and Its Ecological Consequences. Curr. Zool. 2018, 64, 623–630. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Youngsteadt, E.; Keighron, M.C. Urban Pollination Ecology. Annu. Rev. Ecol. Evol. Syst. 2023, 54, 21–42. [Google Scholar] [CrossRef] [Scilit]
  27. Monclús, R.; von Holst, D.; Blumstein, D.T.; Rödel, H.G. Long-Term Effects of Litter Sex Ratio on Female Reproduction in Two Iteroparous Mammals. Funct. Ecol. 2014, 28, 954–962. [Google Scholar] [CrossRef] [Scilit]
  28. Dahlbäck, M.; Andersson, M. Biology of the Wild Rabbit, Oryctolagus cuniculus, in Southern Sweden. IV. Leydig Cell Activity and Seasonal Development of Two Male Accessory Organs of Reproduction. Acta Zool. 1981, 62, 113–120. [Google Scholar] [CrossRef] [Scilit]
  29. Bell, D.J.; Webb, N.J. Effects of Climate on Reproduction in the European Wild Rabbit (Oryctolugus cuniculus). J. Zool. 1991, 224, 639–648. [Google Scholar] [CrossRef] [Scilit]
  30. Armour, C.J.; Thompson, H.V. Spread of Myxomatosis in the First Outbreak in Great Britain. Ann. Appl. Biol. 1955, 43, 511–518. [Google Scholar] [CrossRef] [Scilit]
  31. Villafuerte, R.; Calvete, C.; Blanco, J.C.; Lucientes, J. Incidence of Viral Hemorrhagic Disease in Wild Rabbit Populations in Spain. Mammalia 1995, 59, 651–660. [Google Scholar] [CrossRef] [Scilit]
  32. Moreno, S.; Villafuerte, R. Traditional Management of Scrubland for the Conservation of Rabbits Oryctolagus cuniculus and Their Predators in Doñana National Park, Spain. Biol. Conserv. 1995, 73, 81–85. [Google Scholar] [CrossRef]
  33. Delibes-Mateos, M.; Farfán, M.Á.; Olivero, J.; Vargas, J.M. Land-Use Changes as a Critical Factor for Long-Term Wild Rabbit Conservation in the Iberian Peninsula. Environ. Conserv. 2010, 37, 169–176. [Google Scholar] [CrossRef] [Scilit]
  34. Bach, H.; Escoubet, H.; Mayer, M. Co-Occurrence Patterns and Habitat Selection of the Mountain Hare, European Hare, and European Rabbit in Urban Areas of Sweden. Mamm. Biol. 2023, 103, 187–203. [Google Scholar] [CrossRef] [Scilit]
  35. Ziege, M.; Babitsch, D.; Brix, M.; Kriesten, S.; Seidemann, A.; Straskraba, S.; Wenninger, S.; Plath, M. Anpassungsfähigkeit des Europäischen Wildkaninchens (Oryctolagus cuniculus) entlang eines rural-urbanen Gradienten. Beiträge Zur Jagd-Und Wildforsch 2013, 38, 189–199. [Google Scholar]
  36. Ziege, M.; Brix, M.; Schulze, M.; Seidemann, A.; Straskraba, S.; Wenninger, S.; Streit, B.; Wronski, T.; Plath, M. From Multifamily Residences to Studio Apartments: Shifts in Burrow Structures of European Rabbits along a Rural-to-Urban Gradient. J. Zool. 2015, 295, 286–293. [Google Scholar] [CrossRef] [Scilit]
  37. Ziege, M.; Bierbach, D.; Bischoff, S.; Brandt, A.L.; Brix, M.; Greshake, B.; Merker, S.; Wenninger, S.; Wronski, T.; Plath, M. Importance of Latrine Communication in European Rabbits Shifts along a Rural-to-Urban Gradient. BMC Ecol. 2016, 16, 29. [Google Scholar] [CrossRef] [Scilit]
  38. Ziege, M.; Hermann, B.T.; Kriesten, S.; Merker, S.; Ullmann, W.; Streit, B.; Wenninger, S.; Plath, M. Ranging Behavior of European Rabbits (Oryctolagus cuniculus) in Urban and Suburban Landscapes. Mammal Res. 2020, 65, 607–614. [Google Scholar] [CrossRef] [Scilit]
  39. Ziege, M.; Babitsch, D.; Brix, M.; Kriesten, S.; Straskraba, S.; Wenninger, S.; Wronski, T.; Plath, M. Extended Diurnal Activity Patterns of European Rabbits along a Rural-to-Urban Gradient. Mamm. Biol. 2016, 81, 534–541. [Google Scholar] [CrossRef] [Scilit]
  40. Prinzinger, R.; Misovic, A. Ontogeny of Blood Parameters in the Domestic Fowl Gallus Gallus Domesticus: II. Plasma Parameter. J. Vet. Sci. Med. Diagn. 2015, 4, 1–8. [Google Scholar] [CrossRef]
  41. Cattadori, I.M.; Boag, B.; Hudson, P.J. Parasite Co-Infection and Interaction as Drivers of Host Heterogeneity. Int. J. Parasitol. 2008, 38, 371–380. [Google Scholar] [CrossRef] [Scilit]
  42. Augusteyn, R.C. On the Relationship between Rabbit Age and Lens Dry Weight: Improved Determination of the Age of Rabbits in the Wild. Mol. Vis. 2007, 13, 2030–2034. [Google Scholar] [PubMed]
  43. Frank, R.; Kuhn, T.; Mehlhorn, H.; Rueckert, S.; Pham, D.; Klimpel, S. Parasites of Wild Rabbits (Oryctolagus cuniculus) from an Urban Area in Germany, in Relation to Worldwide Results. Parasitol. Res. 2013, 112, 4255–4266. [Google Scholar] [CrossRef] [Scilit]
  44. Virgós, E.; Cabezas-Díaz, S.; Malo, A.; Lozano, J.; López-Huertas, D. Factors Shaping European Rabbit. Acta Theriol. 2003, 48, 113–122. [Google Scholar] [CrossRef] [Scilit]
  45. Sneddon, I.A. Latrine Use by the European Rabbit (Oryctolagus cuniculus). J. Mammal. 1991, 72, 769–775. [Google Scholar] [CrossRef] [Scilit]
  46. Sibilia, M. Endoparasiten Beim Europäischen Wildkaninchen (Oryctolagus cuniculus L.) in Abhängigkeit von Alter, Geschlecht, Gewicht, Geburtsjahr, Sterbesaison, Wurfgröße und Sozialstatus des Muttertieres. Diploma Thesis, Veterinärmedizinische Universität Wien, Wien, Austria, 2008. [Google Scholar]
  47. Kessel, J.F.; Jankiewicz, A. Species Differntiation of the Coccidia of the Domestic Rabbit Based on a Study of the Oöcysts. Am. J. Epidemiol. 1931, 14, 304–324. [Google Scholar] [CrossRef] [Scilit]
  48. Bush, A.O.; Lafferty, K.D.; Lotz, J.M.; Shostak, A.W. Parasitology Meets Ecology on Its Own Terms: Margolis et Al. Revisited. J. Parasitol. 1997, 83, 575–583. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  49. Kalbe, M.; Wegner, K.; Reusch, T. Dispersion Patterns of Parasites in 0+ Year Three-Spined Sticklebacks: A Cross Population Comparison. J. Fish Biol. 2002, 60, 1529–1542. [Google Scholar] [CrossRef] [Scilit]
  50. Begon, M.E.; Harper, J.L.; Townsend, C.R. Ecology, 3rd ed.; Blackwell Science: Oxford, UK, 1996. [Google Scholar]
  51. Moore, D.M.; Zimmerman, K.; Smith, S.A. Hematological Assessment in Pet Rabbits: Blood Sample Collection and Blood Cell Identification. Vet. Clin. North Am. Exot. Anim. Pract. 2015, 18, 9–19. [Google Scholar] [CrossRef] [Scilit]
  52. Tousson, E.; El-Moghazy, M.; El-Atrsh, E. The Possible Effect of Diets Containing Nigella sativa and Thymus vulgaris on Blood Parameters and Some Organs Structure in Rabbit. Toxicol. Ind. Health 2011, 27, 107–116. [Google Scholar] [CrossRef] [Scilit]
  53. Ajayi, A.F. Haematological and Serum Biochemical Indices of Pre-Pubertal Male Rabbits Fed with Graded Level of Blood-Wild Sunflower Forage Meal Mixture. Afr. J. Biotechnol. 2012, 11, 8730–8734. [Google Scholar] [CrossRef] [Scilit]
  54. Marín-García, P.J.; Llobat, L. What Are the Keys to the Adaptive Success of European Wild Rabbit (Oryctolagus cuniculus) in the Iberian Peninsula? Animals 2021, 11, 2453. [Google Scholar] [CrossRef] [Scilit]
  55. Partridge, G.G.; Findlay, M.; Garthwaite, P.H. Protein and Energy Retention by Growing Rabbits Offered Diets with Increasing Proportions of Fibre. J. Agric. Sci. 1989, 112, 171–178. [Google Scholar] [CrossRef] [Scilit]
  56. Fernández, C.; Fraga, M.J. Effect of fat inclusion in diets for rabbits on the efficiency of digestible energy and protein utizilation. World Rabbit Sci. 2010, 4, 19–23. [Google Scholar] [CrossRef] [Scilit]
  57. Ryan, A.M.; Partan, S.R. Urban Wildlife Behavior. In Urban Wildlife Conservation—Theory and Praxis; Springer Nature: Berlin, Germany, 2014; pp. 149–173. [Google Scholar]
  58. Snell-Rood, E.C.; Wick, N. Anthropogenic Environments Exert Variable Selection on Cranial Capacity in Mammals. Proc. R. Soc. B Biol. Sci. 2013, 280, 20131384. [Google Scholar] [CrossRef] [Scilit]
  59. Ziege, M.; Theodorou, P.; Jüngling, H.; Merker, S.; Plath, M.; Streit, B.; Lerp, H. Population Genetics of the European Rabbit along a Rural-to-Urban Gradient. Sci. Rep. 2020, 10, 2448. [Google Scholar] [CrossRef] [Scilit]
  60. Delgado-V, C.A.; French, K. Parasite-Bird Interactions in Urban Areas: Current Evidence and Emerging Questions. Landsc. Urban Plan. 2012, 105, 5–14. [Google Scholar] [CrossRef] [Scilit]
  61. Thamm, S.; Kalko, E.K.V.; Wells, K. Ectoparasite Infestations of Hedgehogs (Erinaceus europaeus) Are Associated with Small-Scale Landscape Structures in an Urban-Suburban Environment. Ecohealth 2009, 6, 404–413. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  62. Shepherd, R.C.H.; Edmonds, J.W. Observations of ectoparasites of the wild rabbit Oryctolagus cuniculus (L.) in the werribee district of Victoria. Aust. J. Entomol. 1973, 12, 195–200. [Google Scholar] [CrossRef] [Scilit]
  63. Tenquist, J.D.; Charleston, W.A.G. A Revision of the Annotated Checklist of Ectoparasites of Terrestrial Mammals in New Zealand. J. R. Soc. N. Z. 2001, 31, 481–542. [Google Scholar] [CrossRef] [Scilit]
  64. Boag, B. Observations on the Seasonal Incidence of Myxomatosis and Its Interactions with Helminth Parasites in the European Rabbit (Oryctolagus cuniculus). J. Wildl. Dis. 1988, 24, 450–455. [Google Scholar] [CrossRef] [Scilit]
  65. Audebert, F.; Cassone, J.; Hoste, H.; Durette-Desset, M.C. Morphogenesis and Distribution of Trichostrongylus retortaeformis in the Intestine of the Rabbit. J. Helminthol. 2000, 74, 95–107. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  66. Eira, C.; Torres, J.; Miquel, J.; Vingada, J. The Helminth Parasites of the Wild Rabbit Oryctolagus cuniculus and Their Effect on Host Condition in Dunas de Mira, Portugal. J. Helminthol. 2007, 81, 239–246. [Google Scholar] [CrossRef] [Scilit]
  67. Coudert, P.; Licois, D.; Provôt, F.; Drouet-Viard, F. Eimeria Sp. from the Rabbit (Oryctolagus cuniculus): Pathogenicity and Immunogenicity of Eimeria Intestinalis. Parasitol. Res. 1993, 79, 186–190. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  68. Munday, B.L.; Smith, D.D.; Frenkel, J.K. Sarcocystis and Related Organisms in Australian Wildlife: IV. Studies on Sarcocystis Cuniculi in European Rabbits (Oryctolagus cuniculus). J. Wildl. Dis. 1980, 16, 201–204. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  69. Mohamed, H.A.; Molyneux, D.H. In Vitro Cultivation of Herpetosoma trypanosomes in Insect Cell Tissue Culture Media. Parasitol. Res. 1987, 73, 9–14. [Google Scholar] [CrossRef] [Scilit]
  70. Hadfield, S.J.; Chalmers, R.M. Detection and Characterization of Cryptosporidium cuniculus by Real-Time PCR. Parasitol. Res. 2012, 111, 1385–1390. [Google Scholar] [CrossRef] [Scilit]
  71. Mathis, A.; Åkerstedt, J.; Tharaldsen, J.; Ødegaard; Deplazes, P. Isolates of Encephalitozoon Cuniculi from Farmed Blue Foxes (Alopex Lagopus) from Norway Differ from Isolates from Swiss Domestic Rabbits (Oryctolagus cuniculus). Parasitol. Res. 1996, 82, 727–730. [Google Scholar] [CrossRef] [Scilit]
  72. Sroka, J.; Zwoliński, J.; Dutkiewicz, J.; Tós-Luty, S.; Latuszyńska, J. Toxoplasmosis in Rabbits Confirmed by Strain Isolation: A Potential Risk of Infection among Agricultural Workers. Ann. Agric. Environ. Med. 2003, 10, 125–128. [Google Scholar] [CrossRef] [PubMed]
  73. Boag, B.; Lello, J.; Fenton, A.; Tompkins, D.M.; Hudson, P.J. Patterns of Parasite Aggregation in the Wild European Rabbit (Oryctolagus cuniculus). Int. J. Parasitol. 2001, 31, 1421–1428. [Google Scholar] [CrossRef] [Scilit]
  74. Werner, C.S.; Nunn, C.L. Effect of Urban Habitat Use on Parasitism in Mammals: A Meta-Analysis. Proc. R. Soc. B 2020, 287, 20200397. [Google Scholar] [CrossRef] [Scilit]
  75. Foronda, P.; del Castillo, A.; Abreu, N.; Figueruelo, E.; Piñero, J.; Casanova, J.C. Parasitic Helminths of the Wild Rabbit, Oryctolagus Cuniculus, in Different Bioclimatic Zones in Tenerife, Canary Islands. J. Helminthol. 2003, 77, 305–309. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  76. Smith, K.E.; Wall, R.; Berriatua, E.; French, N.P. The Effects of Temperature and Humidity on the Off-Host Survival of Psoroptes Ovis and Psoroptes Cuniculi. Vet. Parasitol. 1999, 83, 265–275. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Rural sites (light grey): (1) Kriftel (rabbit density, 0.56), (2) Gabsheim, (3) Bechtholsheim, (4) Mainz ZDF, (5) Bad Vilbel (rabbit density, 0.88), (6) Maintal (rabbit density, 0.86), (7) Dreieich. Götzenhain; Suburban sites (mid grey): (8) Grüneburgpark (rabbit density, 0.26), (9) Rebstockpark (rabbit density, 15.02), (10) Miquelanlage (rabbit density, 2.27), (11) Elli-Lucht-Park (rabbit density, 22.50), (12) Ostpark (rabbit density, 19.14); Urban sites (dark grey): (13) Friedberger Anlage (rabbit density, 8.16), (14) Oskar-von-Miller Straße, (15) Deutschherren Ufer, (16) Rotschildpark, (17) Taunusanlage (rabbit density, 4.0), (18) Bockenheimer Anlage (rabbit density, 3.55), (19) Eschenheimer Anlage (rabbit density, 13.95). Rabbits have been caught at sites 1–5 and 13–17, and fecal samples from rabbit latrines have been collected at sites 1, 5, 6, 8–13, and 17–18. For further information on rabbit density, see [35].
Wild 02 00023 g001
Figure 2. Between class analysis (BCA) ordination plot representing organ weight profiles of the different rabbit populations (green = rural, grey = urban). The between-group variance explained by urbanity was 11.17% (Monte-Carlo test: p = 0.0003).
Wild 02 00023 g002
Figure 3. Shannon–Wiener Index of parasite communities in rabbit feces compared amongst rural, suburban, and urban study sites. Kruskal–Wallis test: x2(2) = 16.42, p ≤ 0.001 (**), n = 764, Dunn’s pairwise comparison test with Bonferroni correction: rural vs. suburban: p ≤ 0.001 (***), rural vs. urban: p ≤ 0.001 (***), suburban vs. urban: p = 0.97.
Wild 02 00023 g003
Table 1. Mean ± standard deviation (SD) for all assessed blood parameters in comparison to the clinical references for domestic rabbits according to [51]. * indicates significant differences according to the results of the MANCOVA.
Standard Blood ParameterReference Values for Domestic RabbitsRural
(Mean ± SD)
Urban
(Mean ± SD)
Glucose (mg/dL) *-99.10 ± 47.43123.90 ± 57.57
Hematokrit HK (%) *28.00–48.0036.83 ± 6.6542.65 ± 5.57
Hemoglobin HB (g/dL) *9.40–17.4011.14 ± 2.1012.44 ± 2.13
Size of the erythrocytes (µm)5.00–7.806.40 ± 0.546.37 ± 0.60
Erythrocytes EZ (#cells × 1012/L)4.37–7.43 6.23 ± 1.326.54 ± 1.73
Lymphocytes LZ (#cells/mm3)27,100–122,30053,380 ± 14,47964,439 ± 40,297
Mean corpuscular hemoglobin MCH (pg/cell)18.00–24.0019.19 ± 5.5820.01 ± 5.58
Mean corpuscular hemoglobin concentration MCHC (%)27.00–34.0030.88 ± 5.5429.31 ± 5.65
Mean corpuscular volume MCV (mm3) *50.00–75.0059.92 ± 16.7669.99 ± 23.94
Lymphocytes (%) *32.00–81.0092.23 ± 7.7684.17 ± 9.63
Granulocytes (%)
Pseudoeosinophils * 15.00–60.005.61 ± 7.5412.33 ± 8.06
Basophils0.00–0.840.45 ± 1.320.83 ± 1.83
Eosinophils0.00–2.000.36 ± 0.660.31 ± 0.62
Monocytes (%)0.00–4.000.13 ± 0.430.36 ± 0.76
Table 2. Mean ± Standard Deviation (SD) for the relative organ weights, body length, and energy content of the stomach of rural and urban European rabbits. * indicates significant differences according to the results of the MANCOVA.
Measured Variable
(Organs in % of Body Weight)
Rural
(Mean ± SD)
Urban
(Mean ± SD)
Stomach *3.51 ± 1.095.20 ± 0.96
Intestines *9.49 ± 2.4614.64 ± 15.90
Spleen 0.04 ± 0.010.04 ± 0.02
Liver *2.83 ± 0.353.52 ± 0.63
Right kidney * 0.32 ± 0.040.30 ± 0.04
Left kidney *0.32 ± 0.040.30 ± 0.04
Fat tissue around kidney * 1.26 ± 1.141.07 ± 1.21
Heart *0.38 ± 0.070.47 ± 0.08
Lung * 0.59 ± 0.230.77 ± 0.19
Thymus 0.08 ± 0.050.09 ± 0.07
Brain *0.56 ± 0.090.65 ± 0.12
Body length * (cm)44.39 ± 3.2741.72 ± 3.58
Energy content of stomach (J/g) 17,557.02 ± 849.3617,932.24 ± 1111.04
Table 3. Prevalence, mean intensity, and mean abundance (±SD) of infections with ecto- and endoparasites in rural and urban wild European rabbits.
RuralUrban
ParasitesPrevalence
(in %)
Mean
Intensity
Mean
Abundance
Prevalence
(in %)
Mean
Intensity
Mean
Abundance
Lice33.33--36.84--
Fleas12.121.00 ± 00.12 ± 0.337.891.00 ± 00.08 ± 0.27
Mites54.55--84.12--
Ticks3.031.00 ± 00.03 ± 0.172.63 2.00 ± 00.05 ± 0.32
P. ambiguus69.70595.39 ± 995.63414.97 ± 871.0439.47265.53 ± 488.27102.57 ± 337.50
T. retortaeformis30.30--21.05--
C. denticulata00015.796.17 ± 4.961.03 ± 2.99
G. strigosum24.24--18.42--
Table 4. Prevalence (P), mean intensity (mI), and mean abundance (mA) ± SD of infections with endoparasite eggs in rural, suburban, and urban rabbit latrines.
Parasites RuralSuburbanUrban
number of samples283224273
number unparasitized11713
number of parasites in population 555
Protozoa
Eimeria sp.P [%]95.2995.9892.97
mI ± SD6600.92 ±16,253.394396.91 ± 8016.135691.79 ± 14,907.54
mA ± SD6266.42 ± 15,901.254200.62 ± 7887.025274.81 ± 14,425.72
Helmintha
Cestoda indet.P [%]27.2710.272.20
mI ± SD678.22 ± 675.14700.70 ± 1109.07639.02 ± 844.59
mA ± SD184.97 ± 606.3278.20 ± 425.7714.04 ± 148.06
Nematodes
P [%]13.1311.6115.38
T. retortaeformismI ± SD283.06 ± 305.60173.97 ± 139.30187.28 ± 114.97
mA ± SD36.28 ± 143.9620.19 ± 72.7628.81 ± 81.37
G. strigosumP [%]28.6227.6835.53
mI ± SD204.35 ± 168.00206.46 ± 193.94279.11 ± 244.15
mA ± SD58.54 ± 128.2757.14 ± 137.3398.15 ± 196.58
P. ambiguusP [%]7.072.232.93
mI ± SD445.96 ± 307.61172.76 ± 175.73208.08 ± 112.39
mA ± SD31.53 ± 139.664.63 ± 38.396.10 ± 39.51
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.