Review

Chromosome Evolution in Birds: Molecular Cytogenetics, Comparative Genomics and Whole Genome Assemblies


by
Darren K. Griffin
1,2,*,
Rebecca E. O’Connor
1,
Luciano C. Pozzobon
3,
Worapong Singchat
2,
Kornsorn Srikulnath
2,
Denis M. Larkin
4,
Rafael Kretschmer
3 and
Michael N. Romanov
1,2,5,*
1
School of Natural Sciences, University of Kent, Canterbury, Kent CT2 7NJ, UK
2
Animal Genomics and Bioresource Research Unit (AGB Research Unit), Faculty of Science, Kasetsart University, Chatuchak, Bangkok 10900, Thailand
3
Laboratório de Citogenética e Evolução, Departamento de Genética, Instituto de Biociências, Universidade Federal do Rio Grande do Sul, Porto Alegre 91501-970, RS, Brazil
4
Department of Comparative Biomedical Sciences, Royal Veterinary College, University of London, London NW1 0TU, UK
5
L. K. Ernst Federal Research Center for Animal Husbandry, Dubrovitsy, Podolsk Urban Okrug, Moscow 142132, Russia
*
Authors to whom correspondence should be addressed.
Encyclopedia 2026, 6(6), 130; https://doi.org/10.3390/encyclopedia6060130
Submission received: 17 March 2026 / Revised: 2 June 2026 / Accepted: 10 June 2026 / Published: 11 June 2026
(This article belongs to the Section Biology & Life Sciences)

Abstract

Contemporary iterations of avian phylogenies based on multiple genome sequence assemblies assign three major clades: Palaeognathae (mostly ratite birds), Galloanseres (land and waterfowl) and the largest group—Neoaves. The latter two are sister clades representing subdivisions of Neognathae, while Neoaves further subdivide into Columbaves (pigeons/doves/cuckoos/bustards, etc.), Mirandornithes (flamingos/grebes), Telluraves (“higher land birds”, including finches) and the newly recognized Elementaves (e.g., penguins/pelicans/hummingbirds/swifts/cranes/shorebirds). Molecular studies provide clade information, likely divergence timings and a framework from which gross genomic (chromosomal) changes may be mapped. In this review, we consider the patterns of chromosome change that have occurred throughout all avian clades thus far examined, citing studies from standard karyotyping through molecular cytogenetics to whole genome assemblies. Standard karyotyping led to the realization that most chromosomes (particularly the microchromosomes and dot chromosomes) could not be distinguished by classical means. Indeed, cross-species comparisons were difficult, even among the macrochromosomes, because of indistinct banding patterns. Based on fluorescence (or fluorescent) in situ hybridization (FISH), comparative genomics was thence progressed considerably by cross-species chromosome painting (Zoo-FISH) for the macrochromosomes and interspecific mapping of bacterial artificial chromosome (BAC) probes for the microchromosomes. A key finding was that the most studied species, the chicken, fortuitously, has a genomic organization somewhat akin to that of the ancestral karyotype and tends to be the standard from which all others are measured. A notable exception is the fusion of basal chromosome 4 with a smaller chromosome that convergently appears in some other Galliformes, at least one goose and one dove species. While some groups such as Falconiformes (falcons, etc.) and Psittaciformes (parrots, etc.) underwent extensive interchromosomal change, most, broadly speaking, retain a basic karyotype that differs little from bird to bird. Many, e.g., Passeriformes (finches, songbirds, etc.) and Columbiformes (pigeons, doves), do this despite multiple intrachromosomal rearrangements. The complete karyotype and fully established chromosome-level genome assembly of the chicken allow full integration of DNA sequence assembly with karyotype. They further permit cytogenetic studies to be performed using genome assemblies alone alongside cutting-edge long-read sequencing and optical mapping without the need for chromosome preparation. The classic ZW sex-determination system of birds is easily visible in most Neognathae species, but intrachromosomal change in the sex chromosomes is faster than in the autosomes; indeed, there are numerous examples of autosomal fusions and new sex chromosomes formed. Sex chromosomes aside, the classic avian karyotype represents a very successful mode of genome organization established before the emergence of the dinosaurs and perpetuated to this day in their only living descendants.

Graphical Abstract

1. Avian Phylogeny

For us to consider the chromosomal evolution of the whole of the class Aves, it needs to be performed in the context of a contemporary phylogenetic tree. It is generally accepted that whole genome sequencing provides the most reliable raw data for the construction of such a tree and, since Jarvis et al. [1] drew the first of these based on multiple avian genome data, there have been numerous alterations and reorganizations. A study by Stiller et al. [2] refined avian phylogeny by focusing on ultraconserved elements, exonic and intronic sequences using over 300 sequenced avian genomes. This approach enabled the removal of bias towards highly conserved elements, while using a relatively small number of samples from previous studies. It also increased the resolution of the resulting tree, the most recent version of which can be found on such web resources as AviList [3] and Avitaxonomicon [4].
Results confirm the subclassification into Palaeognathae (ratites and tinamous) and Neognathae, the latter breaking down into the sister groups Galloanserae (land and waterfowl) and Neoaves (the remainder) [1,2]. Neoaves are thus considered the third and greatest major clade of extant birds comprising ~95% of all species [5]. Within the Neoaves, four significant clades exist [2], with the first three being Columbaves (including pigeons, doves, mesites, sandgrouse, cuckoos, turacos and bustards), Mirandornithes (flamingos and grebes) and Telluraves (commonly referred to as “higher land birds”, including Afroaves and Australaves (e.g., finches). The fourth is a newly described, very diverse clade called Elementaves, which includes Phaethontimorphae (sunbitterns, tropicbirds and kagu), Strisores (nightbirds, hummingbirds and swifts,), Aequornithes (e.g., pelicans, penguins, loons and tubenoses), Opisthocomiformes (hoatzins), and Cursorimorphae (shorebirds and cranes) [2].
We now have insight that the Palaeognathae–Neognathae divergence was ~100 million years ago (MYA), the Galloanserae–Neoaves divergence ~88 MYA and the separation of ratites and tinamous ~84 MYA [1,2]. Genomic studies, however, imply that tinamous are nested within ratites, being close to the extinct moa, suggesting that ratites are paraphyletic; that is, the absence of flight appeared homoplastically in this group [6]. Galloanserae are further separated into Galliformes (landfowl) and Anseriformes (waterfowl), an event that occurred when the Cretaceous–Paleogene (K–Pg) boundary extinction event happened ~66 MYA [2,4]. Meanwhile, the primary divergences of Neoaves into Columbea and Passerea occurred slightly before the K–Pg event ~67–69 MYA [2,4]. The K–Pg extinction event led to a massive burst of genomic heterogeneity and changes in some molecular evolution patterns, which facilitated the diversification of modern avian life histories [7,8]. Most divergences within Neoaves, however, largely resolved at the ordinal level sometime later, ~50 MYA, and at the basal split of Passeriformes ~39 MYA. The K–Pg event marked a period of abrupt, widespread extinction and drastic climate change, coinciding with the Chicxulub asteroid impact in what is now modern Mexico. This had a profound impact on early bird groups such as Ornithurae, the ancestors of Neornithes [9]. Stiller et al. [2] updated the avian phylogeny based on the analysis of intragenic regions in 363 avian species from 218 taxonomic groups (92% of the total). The authors also go on to discuss that the number and type of sequences sampled have a larger effect on tree construction than taxon sampling alone. Stiller et al. [2] also found a close association with the K–Pg boundary apart from the Mirandornithes and Columbaves. Inevitably, discrepancies in timescales exists from different studies and the reasons for these include different datasets and different algorithms used.
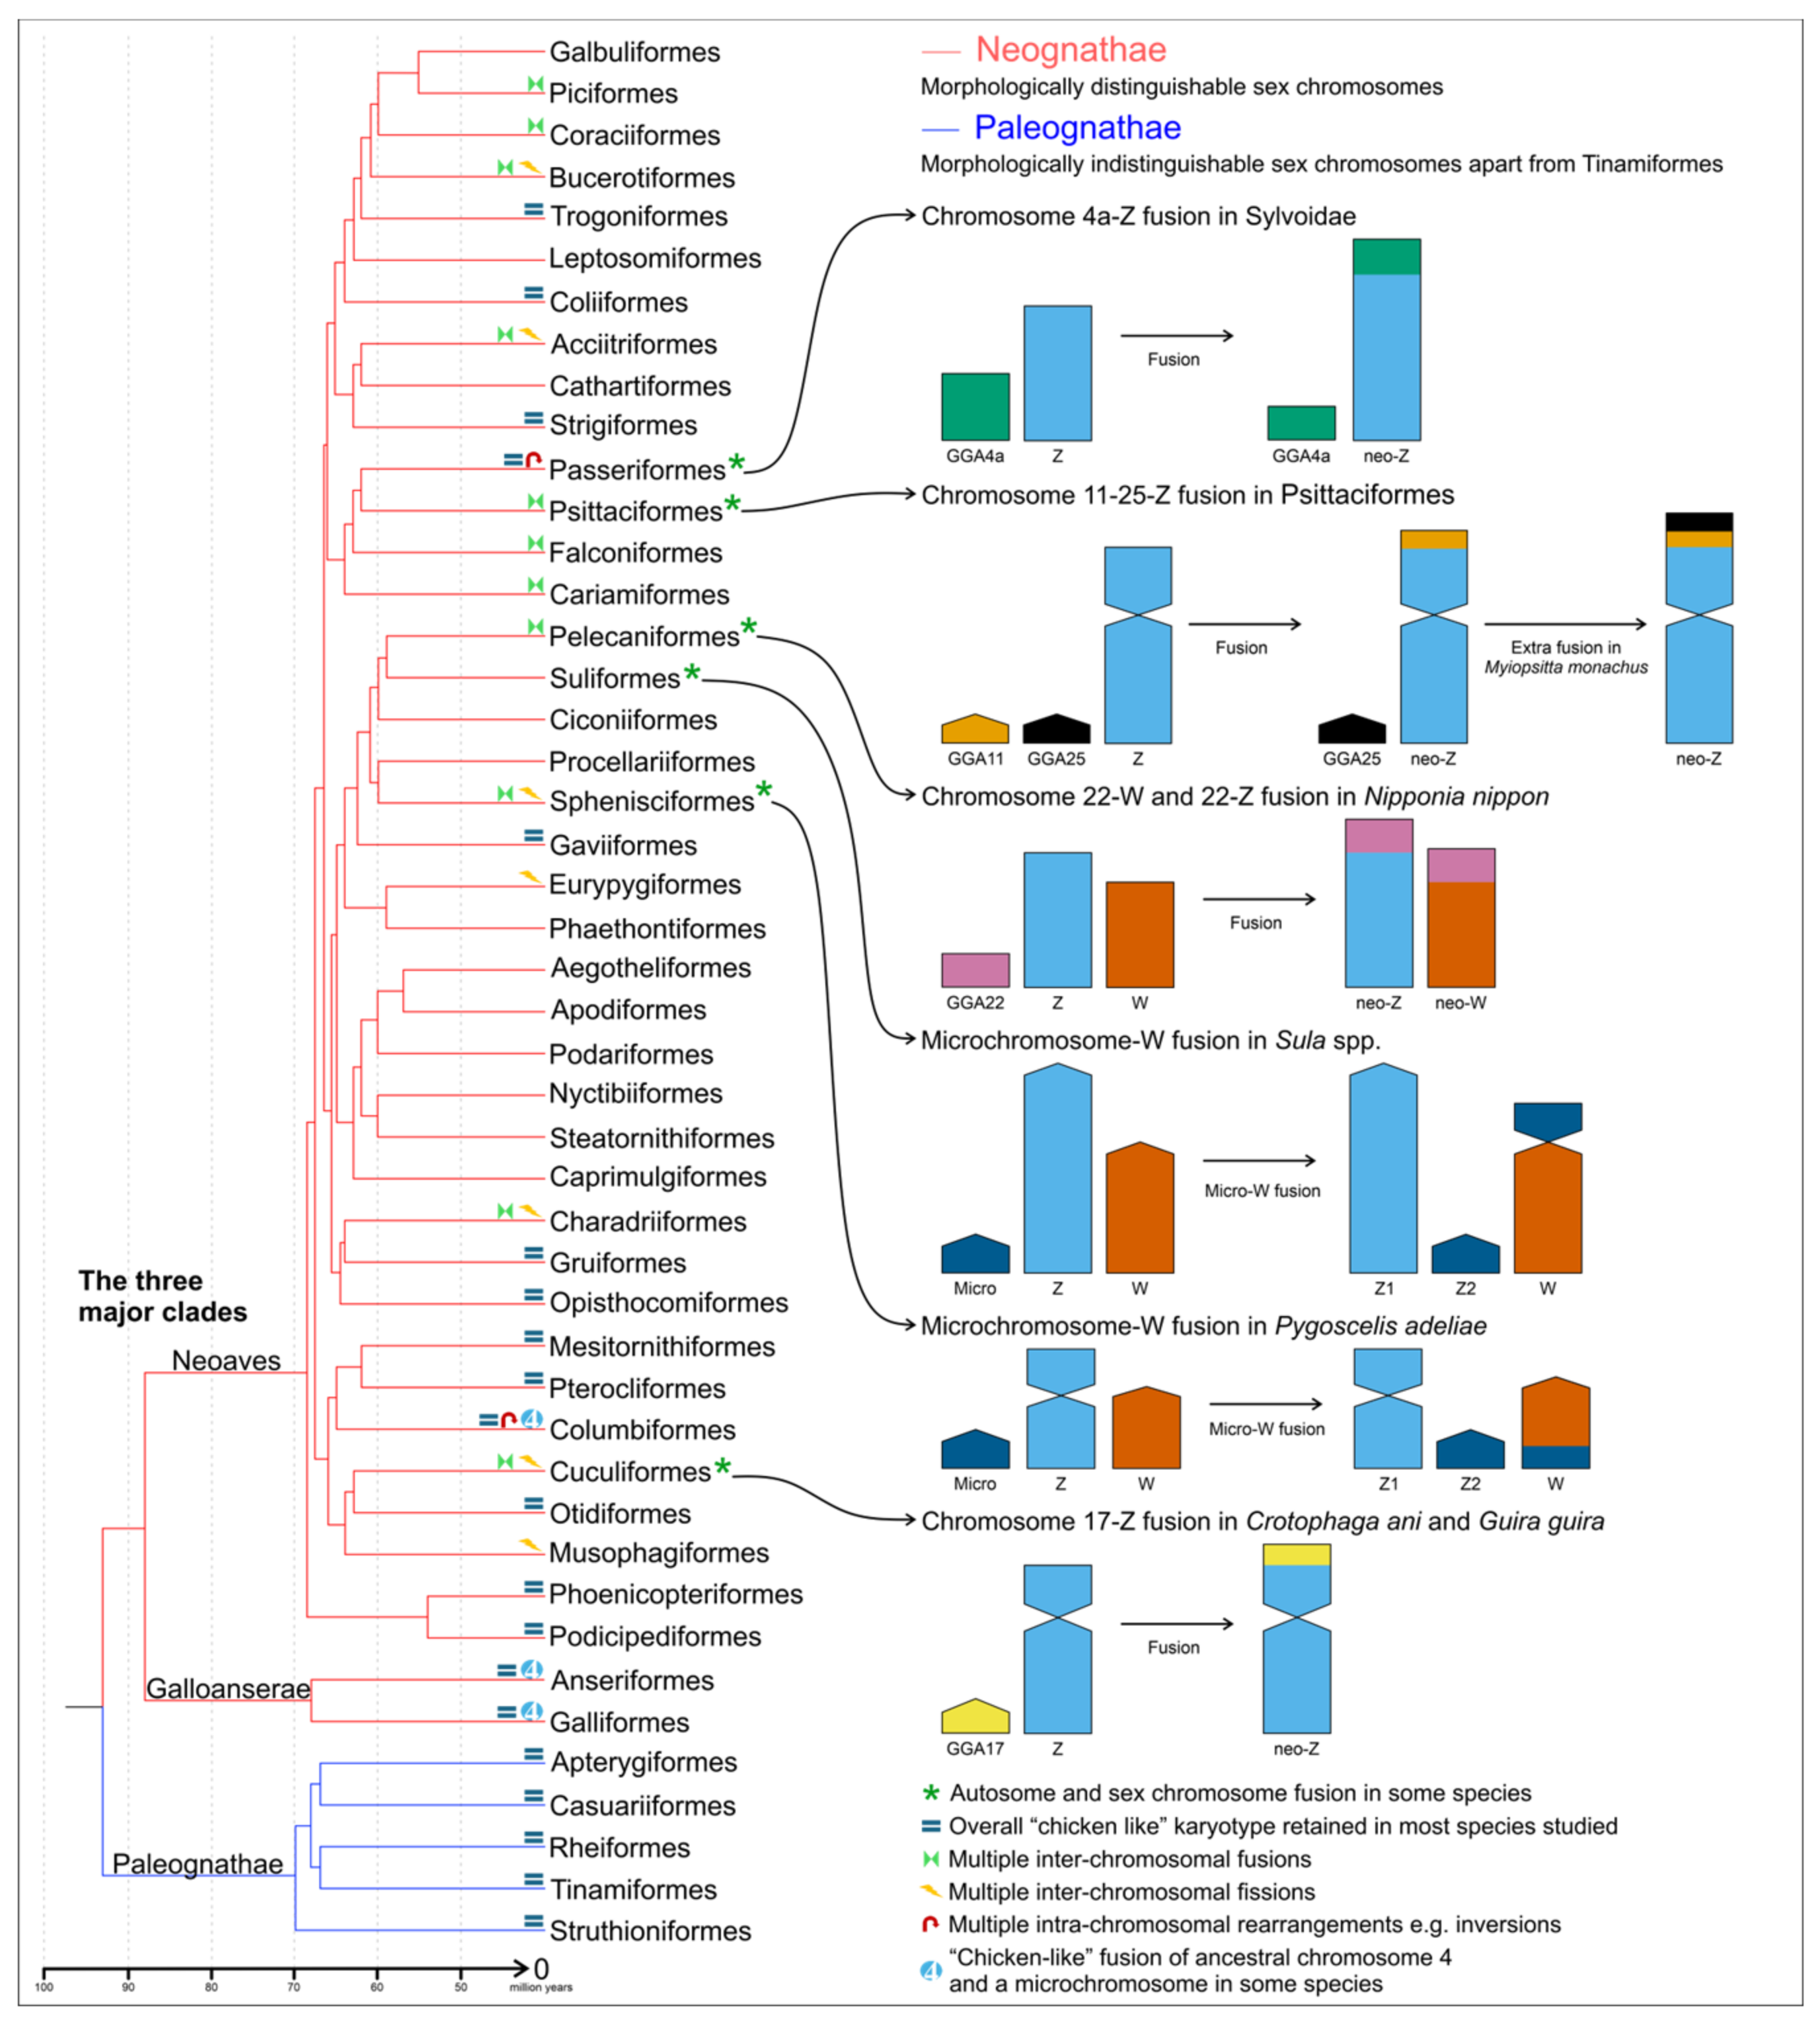
Throughout this review, we will refer to Figure 1, the basis of which is the most recent phylogenetic tree as outlined above. As the various sections unfold, the relevance of the symbols, etc., will become apparent. In all cases, we map the observed changes in overall chromosomal structure (and in that of individual chromosomes) to the phylogenetic tree. Changes are usually made with reference to a universal common avian karyotype, which is very similar to the chicken (Gallus gallus, Galliformes) (e.g., [10]; see also Section 2). A common theme throughout this review is the apparent stability of the avian genome in chromosomal terms (with exceptions) compared to mammalian genomes, which undergo interchromosomal rearrangements far more regularly.

2. Describing the Classical Karyotype of Birds

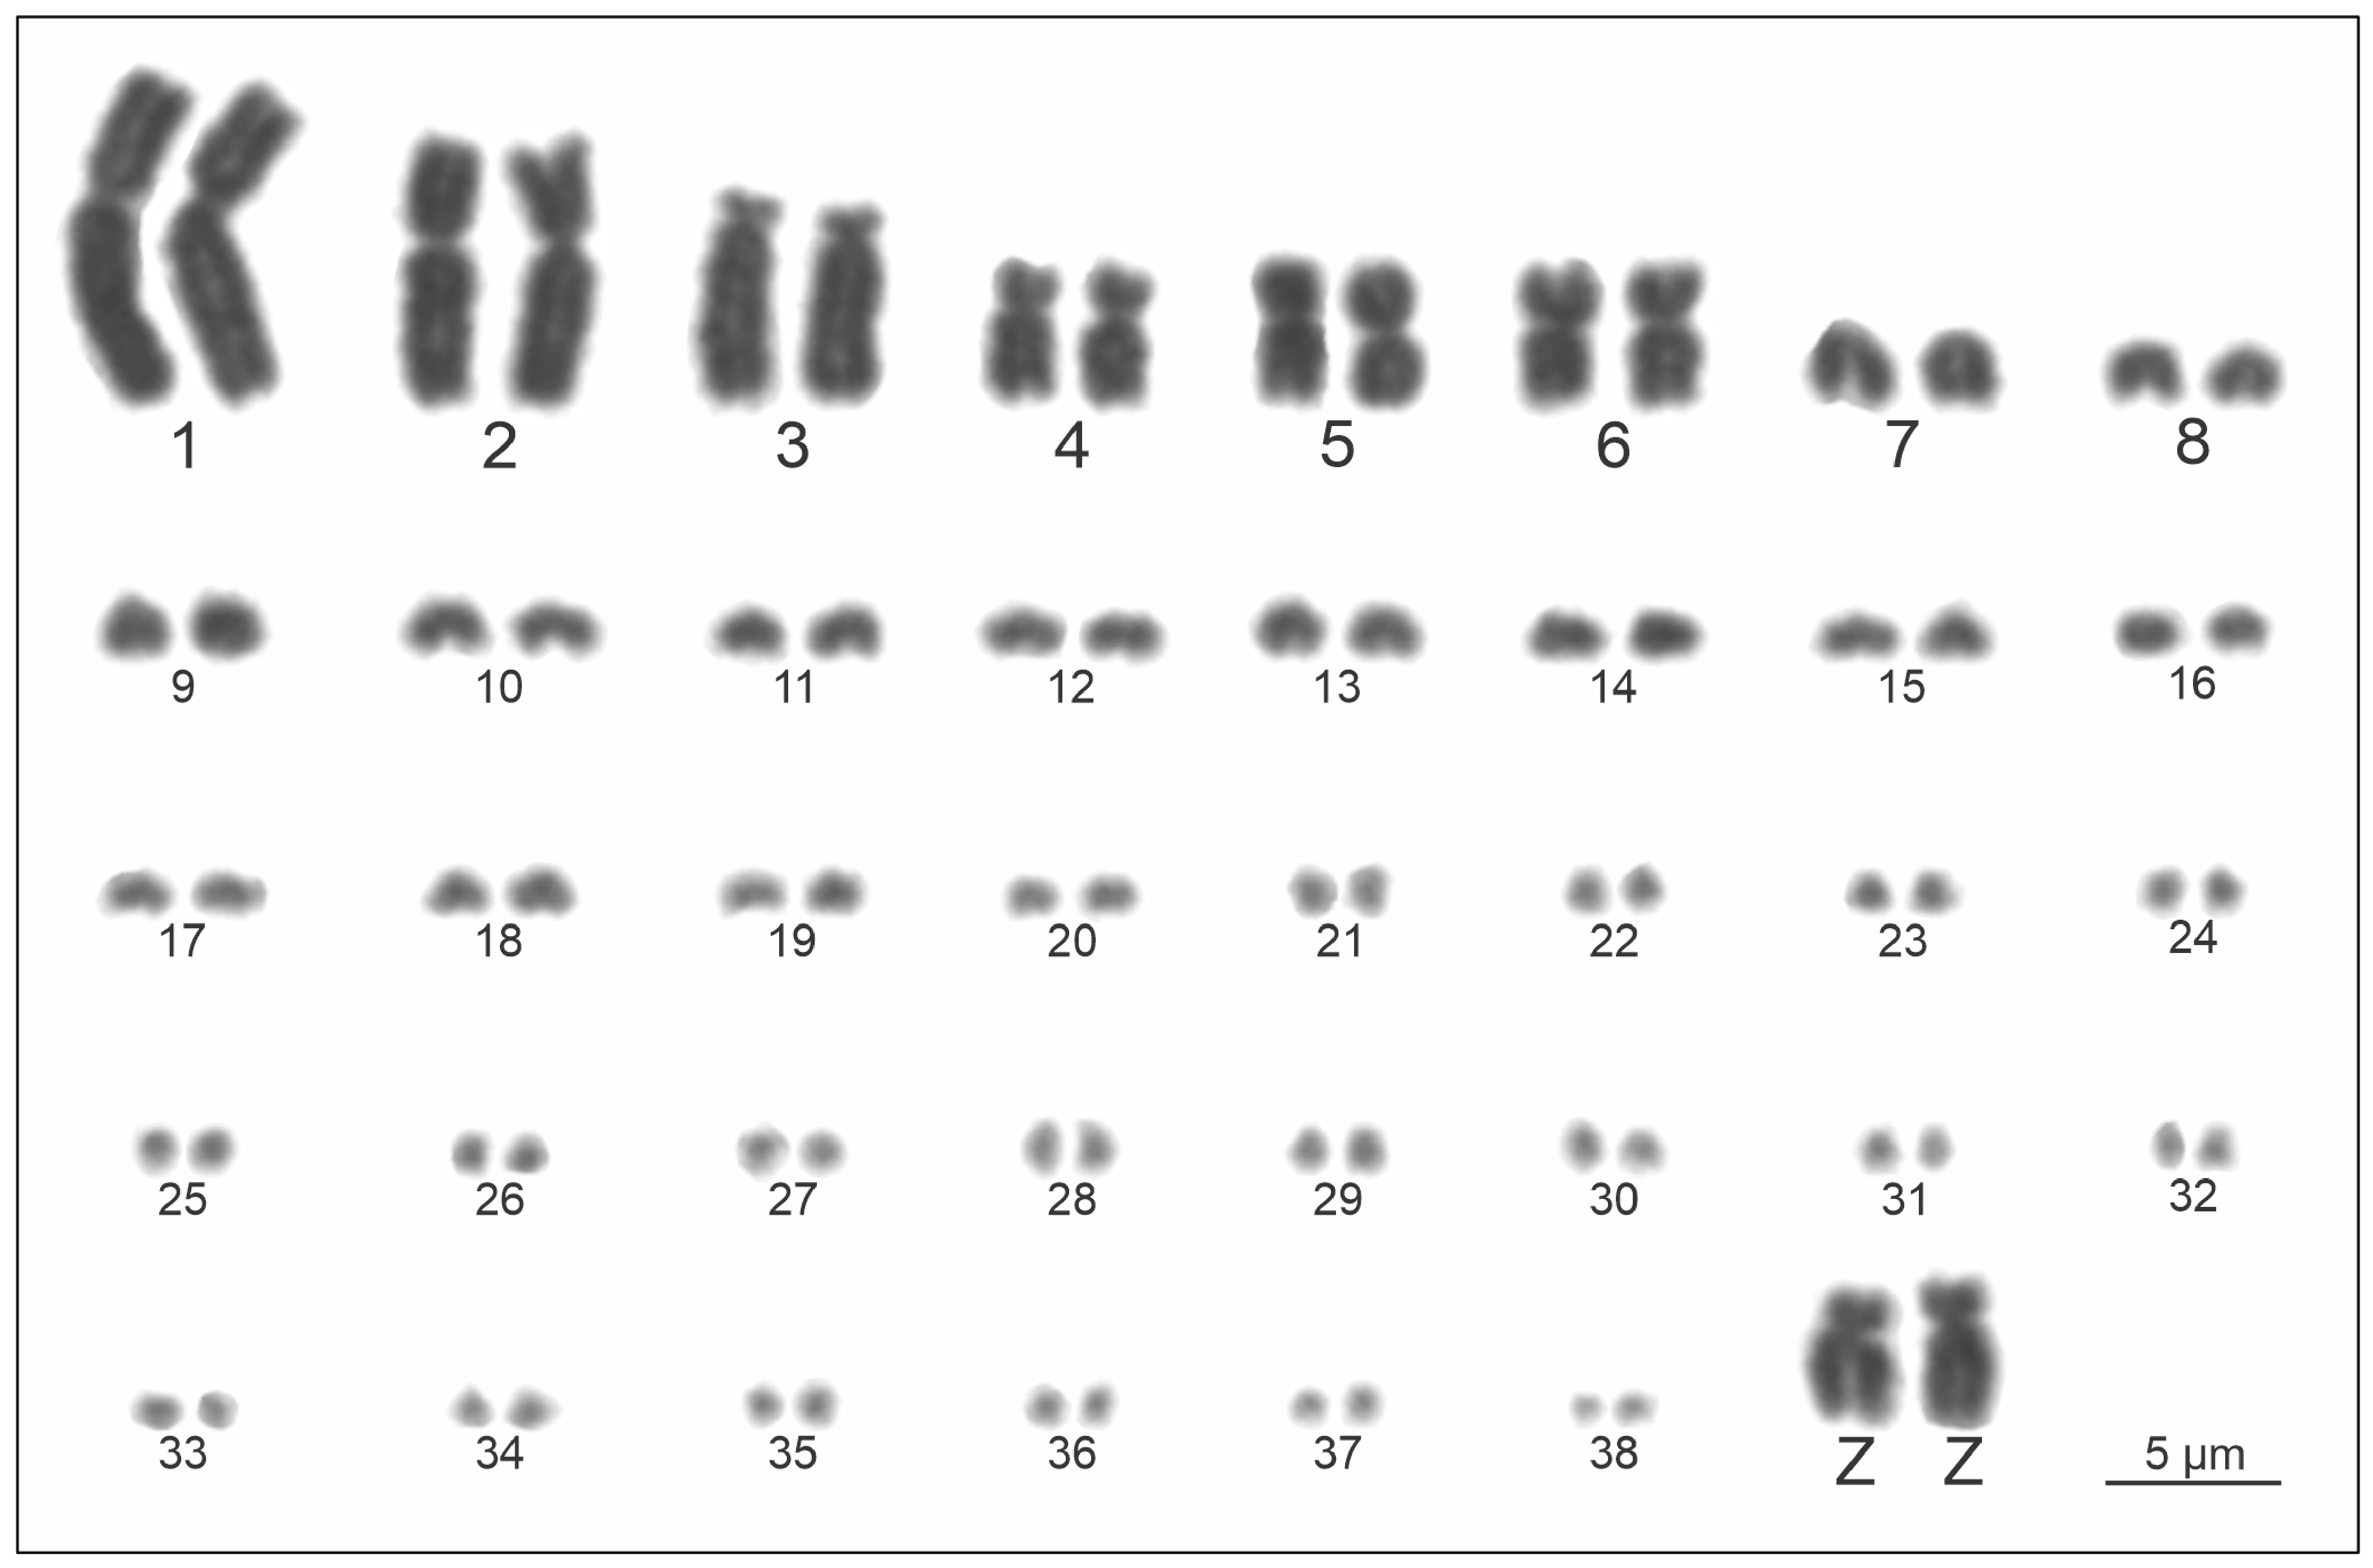
Figure 2 shows a typical avian karyotype, in this case the southern lapwing (Vanellus chilensis, Charadriiformes). In most, or possibly all, avian karyotypes, the chromosomes are subdivided into macro- and microchromosomes. In most (though by no means all) cases, the relative size represents a continuum, and thus different authors may not use the same dividing line between macro- and microchromosomes.
The similarity in the morphology of the microchromosomes, along with their sheer number, makes it near-impossible to distinguish all the chromosomes and thus, although >1200 partial karyotypes of birds have been published [11,12,13], most of these cannot be identified by morphology alone beyond chromosome 10 or even chromosome 5 [14]. Most avian karyotypes, therefore, only identify the largest of chromosomes. With the advent of complete genome assemblies of birds [15], the term “dot chromosome” has been introduced, largely taken to mean the smallest microchromosomes (see later discussion, Section 2.3).

2.1. Chicken: A Near-Ancestral Karyotype from Which All Others Are Measured

The chicken, the most extensively studied avian genome assembly, has a genome size that is approximately 2.8 times smaller than the average mammal [16]. It has a chromosome diploid number of 2n = 78 and is organized into 38 autosome pairs. These include about 9 macrochromosomes (depending on how you do the counting), multiple microchromosomes, and sex chromosomes Z and W; the chicken genome organization is believed to be very similar to the ancestral form of the avian karyotype [17]. Chicken microchromosomes account for about ~23% of the whole genome, but are very gene-rich and, as such, contain at least 50% of the genes [18,19,20,21]. Primitive amphibians and most reptiles also possess microchromosomes, suggesting that many avian microchromosomes reflect archaic vertebrate syntenies [12,13]. Moreover, from a comparative genomic perspective, the conservation of synteny between humans and chickens is greater than that between humans and mice [16].
The karyotype of any species of eukaryote, birds included, fundamentally describes its overall genome structure. It facilitates comparisons of significant genomic differences between species, ultimately helping to draw an evolutionary tree that illustrates gross genomic changes. In chicken, classification of the larger macrochromosomes (up to autosome 9, which also includes the sex chromosomes) [10] was easily accomplished using standard cytogenetic techniques such as chromosome banding and staining [11]; it was nearly impossible, however, below this size. In chicken, therefore, molecular cytogenetic methods were used to define the whole genome [22]. Other birds soon followed, using chicken as a reference.

2.2. Comparative Chromosome Painting in Birds

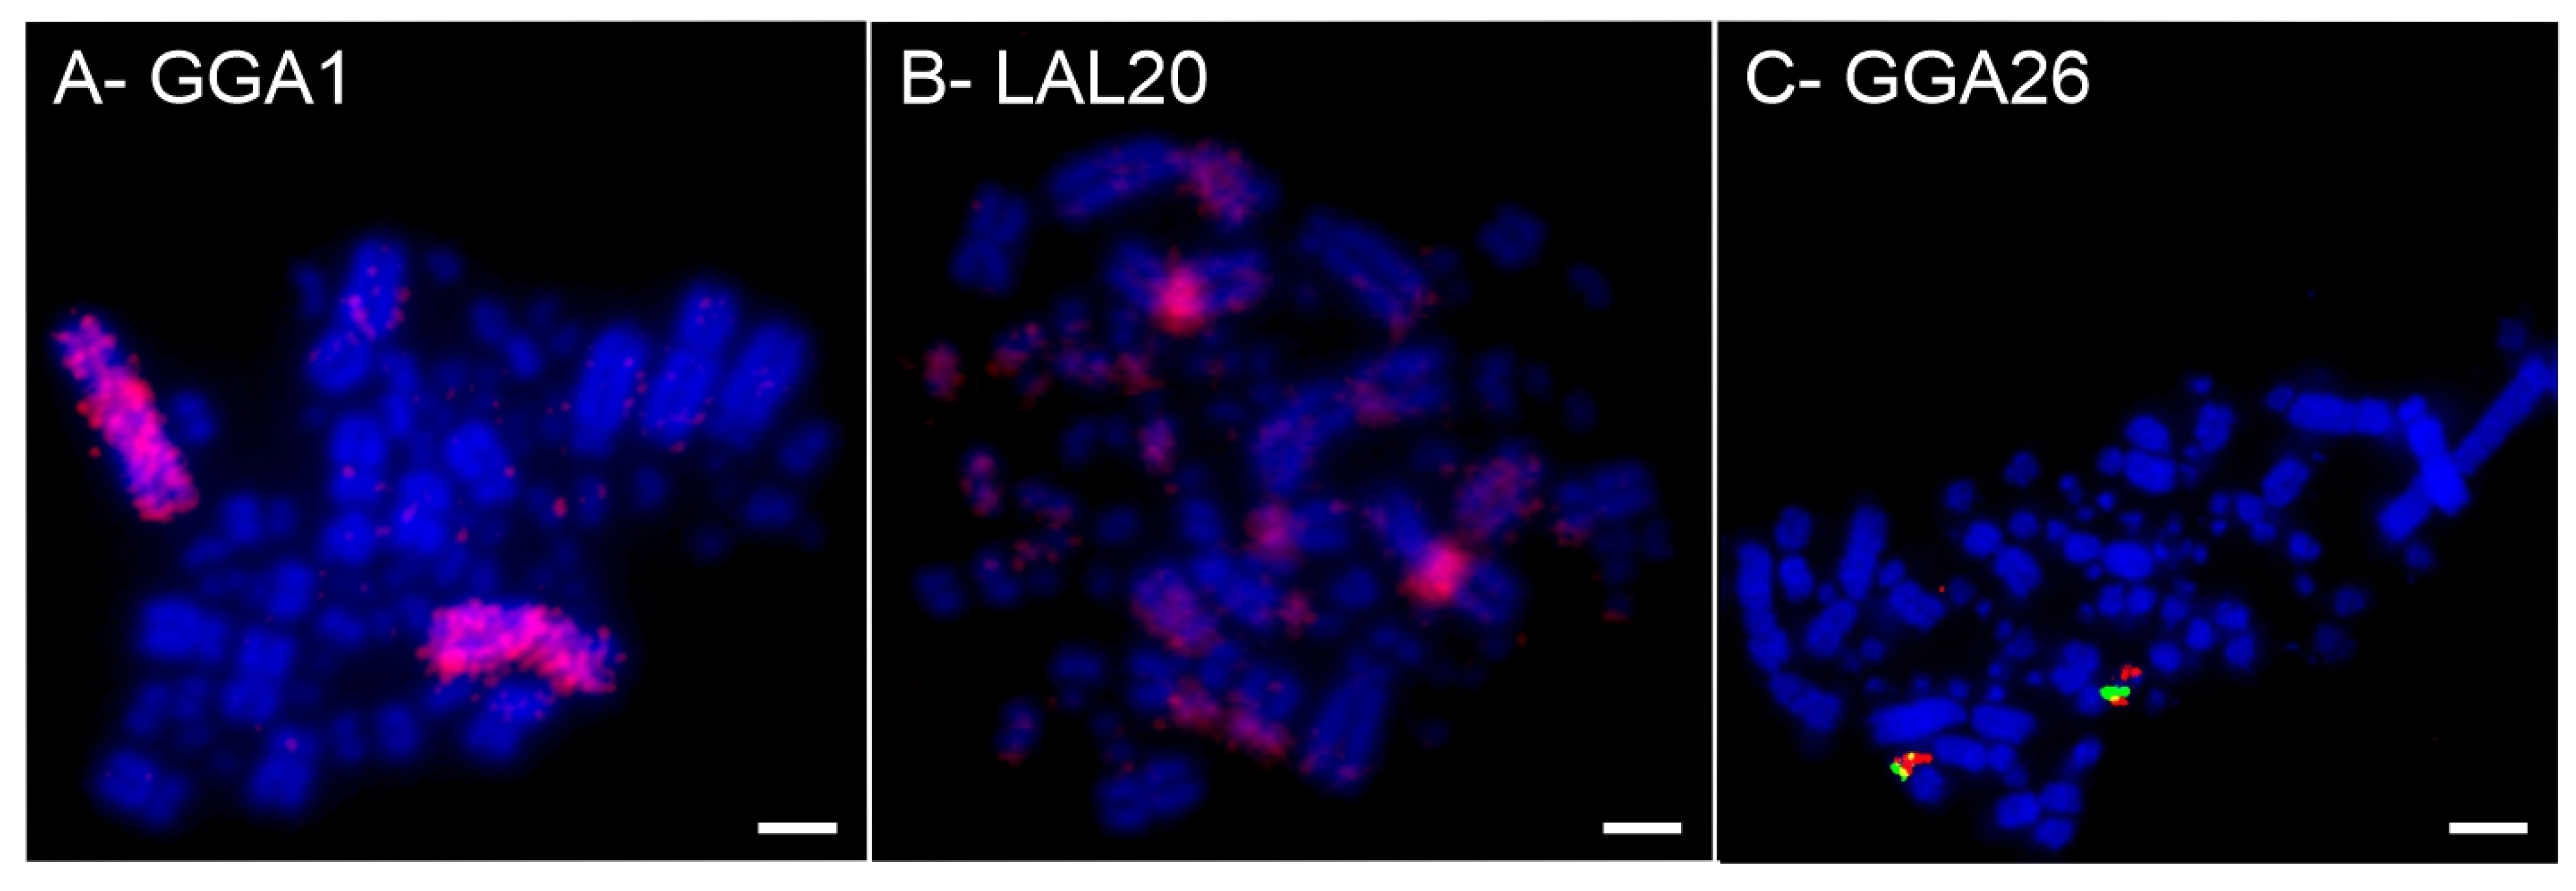
Even at the macrochromosome level, identifying chromosome bands can be difficult, thereby impeding a detailed analysis of cross-species homology. After banding studies, the next level of resolution was through the advent of chromosome paints (e.g., Figure 3A,B). These were created through the amplification and fluorescent labeling of flow-sorted chicken macrochromosomes [23]. Chromosome painting enhanced resolution resulted in cross-species analysis (Zoo-FISH) data that currently encompasses ~120 avian species across ~22 individual orders (reviewed in [13] and in subsequent sections here). Zoo-FISH [24,25] is the term commonly used to refer to the use of chromosome paints generated from one animal species and hybridized to the chromosomes of another to illustrate the evolutionary relationships between them; FISH is an acronym for fluorescence (or fluorescent) in situ hybridization [26].
The primary focus on the larger (macro)chromosomes, however, is due to the abilities of the flow-cytometer to isolate chromosomes up to a certain size. Some progress has been made in generating microchromosomal paints, but this is limited, due to the challenges in separating individual microchromosomes via flow cytometry [22,27]. In this review, we give a synopsis of chromosome painting studies in macrochromosomes; however, we also focus on the microchromosomes and how we are understanding their evolution more than ever using newer approaches. The application of chromosome paints arising from flow-sorted and amplified chicken chromosomes 1–9 + Z revealed a high level of conservation among the macrochromosomes [23]. This supported the notion that overall genome structure (karyotype) in birds is highly conserved, even over considerable phylogenetic distances [11,12,23]. These studies led to a significant increase in bird comparative genomics research, producing results in species as evolutionarily distant from chicken as ostrich (Struthio camelus, Struthioniformes), emu (Dromaius novaehollandiae, Casuariiformes) and falcons (reviewed in [13]). Figure 3A illustrates chromosome painting of chromosome 1 in chicken chromosomes and Zoo-FISH of chicken chromosome 20 onto white hawk (Leucopternis albicollis, Accipitridae) chromosomes (Figure 3B). It also illustrates how two single individual bacterial artificial chromosome (BAC) clones can be used to identify a chicken microchromosome (Figure 3C and see next section).

2.3. Addressing the Microchromosomes

In 2004, the first relatively complete genome sequence of the chicken (Gallus gallus) and the complete definition of its karyotype were published at the same time [16,22]. To identify each microchromosome separately, microchromosome paints were made from microdissected chromosome preparations. However, later efforts to sequence DNA from these clones were technically challenging and ultimately unsuccessful. Additionally, the chromosome paint probes developed by Masabanda et al. [22] have since degraded. Notably, chromosomes 33–39, the smallest microchromosomes, had no corresponding sequences in the genome assembly until recently. As of today, all chicken micro- and macrochromosomes have been assigned sequences and annotated because of the recent efforts of Huang et al. [15], although there were still 172 scaffolds that needed to be assigned at the time of writing. As mentioned at the end of Section 1, these authors also defined the term “dot chromosomes”, singling out 10 specific pairs (chromosomes 16, 29, 30 to 32, 34 to 38) based on their morphology and heterochromatic nature. Broadly, this term is taken to mean the smallest of chromosomes (usually smaller than chromosome 28) and had been previously termed “D group” chromosomes [22].

2.4. Selecting BACs by Bioinformatic Means to Map Evolution of the Microchromosomes

Whilst attempting to define the nature of microchromosomes in avian species by comparison with the domestic chicken, a certain degree of success using a cross-species BAC mapping approach was initially reported [27]. That is, BAC probes that worked well using FISH in chicken experiments were applied to the metaphases of other species. Success was, however, restricted to closely related species, achieving about a 70% success rate when applying chicken BACs to the turkey (Meleagris gallopavo, Galliformes) similar to an estimate [28] established using an OVERGO–BAC hybridization approach (for details, see Section 2.5 and Section 3.4). The success rate dropped to under 40% when tested on the duck (Anas platyrhynchos, Anseriformes) [29,30]. This largely changed, however, with the method of Damas et al. [31], who used BAC libraries from whole genome sequencing efforts and chose a set of BACs that hybridized strongly to all bird microchromosomes and a number of reptiles.
Damas et al. [31] leveraged a bioinformatic approach to identify the unique genomic features of certain BACs, making them suitable for hybridization across multiple species. This dramatically improved hybridization rates between species as selection criteria were based on the proportion of conserved sequences within the BACs. The final selection of individual BACs was based on the successful hybridization to five avian species’ metaphases and their position on the reference species’ chromosomes, specifically targeting the most distal regions of each microchromosome [31]. This strategy provided a reliable point of reference for comparing species and tracking chromosomal rearrangements over time. As Damas et al. [31] reported, this method expanded the scope of comparison from multi-species chromosomal rearrangements within a specific order to comparisons across an entire phylogenetic class, and in some cases, beyond that to other reptiles [32]. The outcome was clear, discrete signals, much like those achieved for chicken metaphases, generated for microchromosomes across each species (curiously, apart from two BACs associated with chicken chromosome 25 when used on Passeriformes). Additionally, distinct signals were generated for all macrochromosome BACs, although there were a few species-specific exceptions [32,33,34].
This set of pan-species probes, specifically targeting microchromosomes (e.g., Figure 3C; but not dot chromosomes as sequences were not available at the time) allowed for analyses at a greater resolution than previously possible. In the majority of studies, two BACs were chosen from each of the chicken microchromosomes that were sequenced (from chicken chromosome 10 to 28, not including 16), with dual FISH conducted on at least 42 avian species to date to the best of our knowledge (reviewed in [13]). In all tested species, regions homologous to Gallus gallus chromosomes 22, 24, 26, and 27 appeared to have remained intact as discrete, solitary microchromosomes, showing no signs of fusion (reviewed in [13]).

2.5. Other Species’ BAC Libraries and OVERGO Hybridization Probes

The application of large-insert BAC libraries for species other than chicken also proved useful for comparative genomic research in birds [35,36,37]. For example, a BAC library for the zebra finch (Taeniopygia guttata, Passeriformes; a model passeriform species) with around 16× coverage was developed by the Arizona Genome Institute, while a library for the emu was created with 13.5× coverage [38,39]. The development of large-insert physical maps for additional avian genome assemblies, aligned with the chicken genome sequence, provided valuable resources [40]. Such comparative maps also enhanced the analysis and application of the latest versions of the chicken genome sequence assembly [15].
One more BAC library hybridization technique involved synthesizing some OVERGO probes by the process of annealing two 22- or 24-base oligonucleotides that had an 8 bp overlap and then labeling them using radiolabeled nucleotides [41,42,43]. OVERGOs generated from regions of high conservation of sequence can be employed to probe new genomes (i.e., those that have not been sequenced) by screening their BAC libraries [44]. Aligning BAC contig maps of other birds against the chicken genomic sequence and creating interspecies comparison maps are just a couple of applications of cross-species OVERGO hybridization. Orthologous BACs from several mammals (including pigs, dogs, cats, cattle and primates) and across vertebrate orders can be found using Universal OVERGO probes, or Uprobes, as shown by the work of Thomas et al. [45]. Investigators can also leverage the database of Uprobes (which is searchable) to achieve cross-species hybridization [46].

2.6. Insertions, Deletions and Duplications

Phylogenetic analyses are based on DNA sequences in other vertebrate classes, such as mammals [47,48], including structural mapping studies [49,50]. The mapping of insertions, deletions and duplications [51,52] established novel pathways for understanding ordinal and familial relationships, providing essential insights and hypotheses that can be tested. A panoply of comparative genomic approaches, including continuous DNA sequence analyses using large-insert genomic libraries [44,53,54], retroposon insertion and other unique genomic changes identification [55,56], offer promising pathways for an integrated understanding of genome evolution. Due to a more equitable representation of repetitive elements in comparison to single-copy DNA elements when compared to mammals, avian genomes present a suitable platform for evaluating these strategies [57]. Furthermore, the genomes of species like the tuatara, American alligator, garter snake, anole lizard and several turtles can serve as reptile outgroups for linking the evolution of avian species with that of reptilian species [58].

2.7. Finally, a Complete Chromosome-Level Assembly

The latest T2T (telomere-to-telomere) chicken genome sequence generated chromosome-scale contigs for all 38 autosomes as well as the Z and W. As little as 26 gaps remain on the W chromosome, mostly found within relatively long stretches of satellite DNA or within simple repeats [15]. Given the hitherto-undiscovered functions of several DNA segments in numerous vertebrate genomes and the dot chromosomes, further comparative research is needed to explore features of genome structure as represented by the karyotype organization. Addressing such issues is now practicable by making use of the newest BAC, fosmid and cosmid libraries [59], FISH, and other techniques to make comparative physical maps with greater coverage [60,61,62,63,64]. Larger sequencing datasets for comprehensive genome analyses, such as conservation-focused studies of avian genomes, can be produced as a result (e.g., [65,66,67,68,69,70,71]). Having a first T2T assembly in one model species has led to T2T assemblies in others and, for instance, revealed that, in the zebra finch T2T genome, non-canonical (non-B) DNA motifs, previously hidden in gaps [72,73], are both markedly enriched on microchromosomes and regulate centromere function [74]. Indeed, the absence of microchromosomal sequences and the consequent gaps in the genome assemblies are now being filled in a series of studies [75,76,77,78].

2.8. Cytogenetics Without Chromosome Preparations

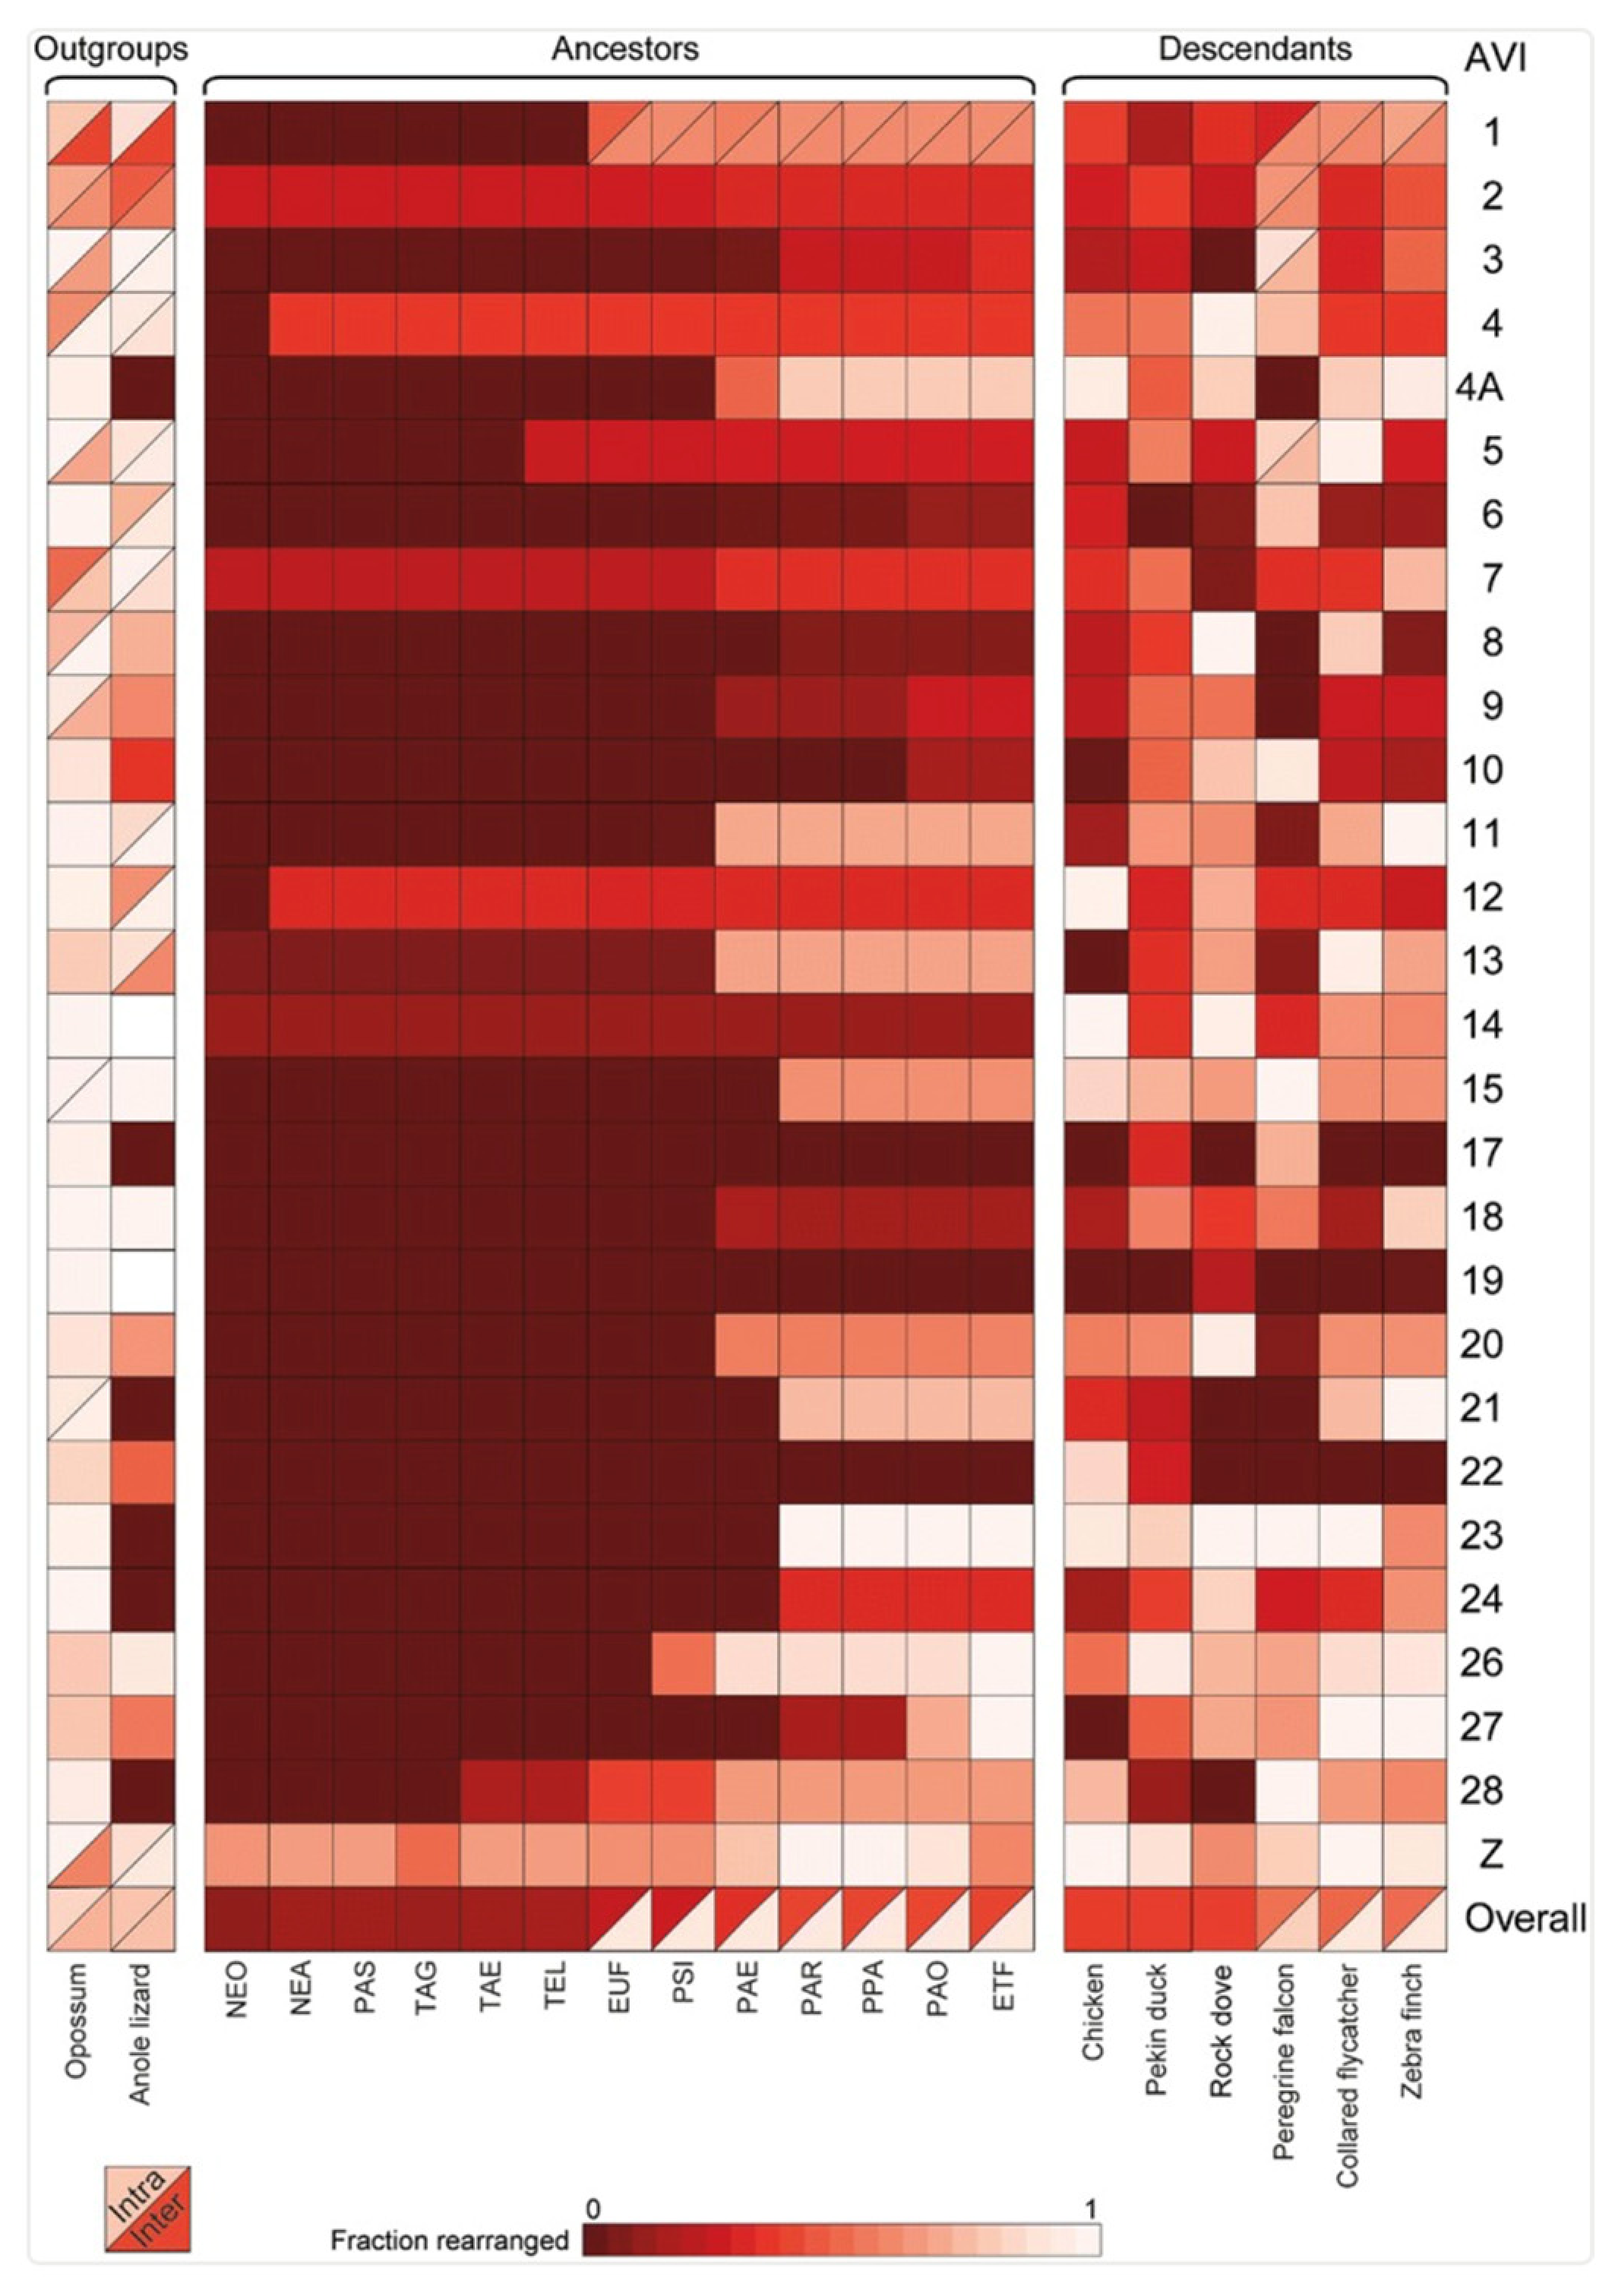
The introduction of novel techniques enabling chromosome-level genome assemblies without the need for chromosome preparations is creating unique opportunities for bird genomic research [79]. This progress is reflected in recent advances in both avian and mammalian genome assemblies. Technologies such as long-read sequencing [80,81], optical mapping [82], and others, including de novo PacBio long-read [83] and phased avian genome assemblies [84,85,86], can enrich reference genomes originally assembled from short- and intermediate-length reads [87,88,89,90,91]. Reads of long to intermediate length have revealed considerable variation in the structure and number of major histocompatibility complex (MHC) loci in avian species [92]. In addition, single-molecule long-read sequencing has established the possible influence of post-transcriptional regulation, which may influence the effects of gene dosage on chromosome Z [93]; optical mapping data have been useful in improving genome assemblies [82,87,94], for instance in the common ostrich [95]. Recent studies of birds have demonstrated that PacBio/single-molecule, real-time (SMRT) long reads [96,97] can uncover evolutionary adaptation and divergence by unraveling the nature of complex genome architectures. An example would be a study by Weissensteiner et al. [98], who put together short- and PacBio long-read data to curate ~220,000 structural variants in corvids, uncovering a ~2.25 kb terminal repeat (LTR) retrotransposon insertion in the NDP gene (encoding the norrin cystine knot growth factor NDP) that, most likely, contributes to premating isolation. In a similar vein, Lundberg et al. [99] used PacBio high-fidelity (HiFi) reads and optical mapping to assemble the genomes of willow warblers, finding three large inversions (0.4–13 Mb) associated with environmental gradients and migratory behavior. Divergence times suggested that these inversions arose in separate refugia and persisted thereafter through hybridization. Zhang et al. [100] assembled eight chromosome-level duck genomes, identified structural variations that differentiate domestic and wild ducks, and showed continuous female-biased gene flow during speciation. These variants appear to affect candidate genes such as the growth hormone receptor (GHR) and FER tyrosine kinase (FER), as well as a large number of LTR retrotransposons reshaping genes, e.g., those encoding insulin-like growth factor 2 mRNA-binding protein 1 (IGF2BP1) and the melanocyte-inducing transcription factor (MITF) in domestication [100]. Collectively, these studies reinforce the notion that high-quality long-read assemblies and genotyping can uncover hidden structural variation and gene flow, thereby providing new insights into adaptive evolution and subsequent speciation of birds. In Figure 4, we illustrate how genome assemblies have been used to detect inter- and intrachromosomal rearrangements from the common ancestor (from [101]). This enables genomicists who are not trained cytogeneticists to interpret chromosomal data using only digital assemblies.

2.9. Avian Sex Chromosomes

Different to mammals, birds carry a conserved ZW sex-determination system, where females are heterogametic (ZW) and males homogametic (ZZ) [11,12,23,102,103]. In all avian species apart from Palaeognathae, the sex chromosomes differ in size and morphology; the W chromosome is mostly heterochromatic, gene-poor, and noticeably smaller than the Z [104]. However, there are exceptions noted in Schartl et al. [105], who summarized that the W chromosome is heterochromatic and comparable in size to (in ostrich, emu, black-winged kite (Elanus caeruleus, Accipitriformes), spectacled owl (Pulsatrix perspicillata, Strigiformes), and common potoo (Nyctibius griseus, Nyctibiiformes)), or even larger than, the Z chromosome (in crimson finch (Neochmia phaeton, Passeriformes) and Indian pond heron (Ardeola grayii, Pelecaniformes)). In ratites, the W chromosome is very close to the size of the Z, and is mostly homologous, with the exception of a tiny pericentric region in emus [105].
It has been proposed that changes in chromatin conformation because of transposable element (TE) accumulation represent an important primary step in the differentiation of the ZW sex chromosomes [106]. Despite the differences in sizes, it is inferred that the ZW system existed before the divergence of Palaeognathae and Neognathae, with the differentiation between the two chromosomes occurring later in evolutionary time [107]. Even though the ZW system, on the face of it, appears to be similar to the XY system in mammals, the XX/XY (mammal) and ZZ/ZW (bird) systems have no homology and therefore arise from entirely separate origins [108]. The avian Z chromosome has homology with the chromosomes 5, 9, and 18 in humans; on the other hand, the human X chromosome has homology with a part of the long arm (or q arm) of chromosome 1 in chicken, as well as a 20 Mb part of the short arm (or p arm) of chromosome 4 in chicken (which is a small chromosome in other avian species’ karyotypes) [13].
The sex-determining locus in avian species is not that for sex-determining region Y (SRY), as appears in mammals (the homolog of SRY is, in fact, found on chromosome 4 in chicken). Instead, the gene for “doublesex and mab-3-related transcription factor 1” (DMRT1), found on chromosome Z, is thought to play a crucial role in sex determination by way of a dosage-dependent mechanism. Male sex determination needs two copies of this gene, as it is found in ZZ males, and DMRT1 is also a key gene for testis development. There remains substantial debate with regard to the mechanisms of sex determination in birds, with several candidates—including W-specific genes—that may affect ovarian function. Progress in the Z chromosome assembly has been made using a BAC-based approach, alongside ongoing efforts to enrich the W chromosome assembly [108,109,110].

2.10. Germline-Restricted Chromosomes (GRCs)

GRCs are supernumerary chromosomes (resembling B chromosomes) and are seen only in the germ cells. They are notable for their variable presence (or indeed absence) among species and for being somewhat dispensable. Although B chromosomes are often noted in plants, animals and fungi, they are not reported in birds. In contrast, GRCs have been seen in all songbirds thus far described, suggesting an ancient, conserved presence that arose about 50 MYA. Despite this, GRCs are highly variable in size and gene content between species [111,112]. In molecular biological terms, they are very dynamic with few similarities compared to autosomes and sex chromosomes [113,114,115]. They are both DNA-repeat-rich and gene-poor, perhaps more like the W chromosome than any other in the karyotype [116,117]. Their variability and evolutionary instability, however, exceeds even that of the W [79,118]. Such peculiar characteristics and possible roles in genome plasticity, as well as germline–soma differentiation, add to the overall picture of avian chromosome evolution.

2.11. Lampbrush Chromosomes

Lampbrush chromosomes are meiotic bivalents that are far larger than regular metaphase chromosomes. They have been an outstanding model system for the study of chromatin organization and RNA synthesis for more than a hundred years [119]. Their highly decondensed nature means that small evolutionary rearrangements and gene order can be studied at high resolution using chromosome painting and/or BAC mapping. One example is that of neocentromere formation on the Japanese quail (Coturnix japonica, Galliformes) chromosome 4, which was detected using BAC–FISH mapping of chicken and quail lampbrush chromosomes [120]. The findings were that the centromeres of chicken and quail chromosomes 4 apparently formed independently to one another after centric fusion of the ancestral chromosome 4 with a large microchromosome. Combining immunolabeling with antibodies raised against subunits of cohesin, Krasikova et al. [121] demonstrated that cohesin-enriched structures, akin to centromeric protein bodies, are characteristic of lampbrush chromosomes in chicken and quail. Up to the present, lampbrush chromosomes are being used in the study of the role of transcription in genome organization of birds and other vertebrates [119].

3. Comparative Cytogenomic Analysis of Birds

The chicken genome sequence (and, to some degree, that of the zebra finch) serves as a reference for comparative mapping, compensating for the limited genetic and genomic knowledge available for many other bird species [122]. The relevance of chickens in the fields of developmental biology and agriculture, and of zebra finch in the fields of developmental biology and neuroscience, ensures that these fundamental reference species’ genomes continue to be well described in functional and molecular terminology [123,124]. These references facilitate addressing broader biological questions pertaining to avian genomes (and that of vertebrate genomes generally) more effectively [125]. Although significant progress has been made in this regard, it is still relatively underdeveloped compared to advancements in mammalian cytogenomics [48,126,127].

3.1. Fast and Slow

Although bird karyotypes evolve at slower rates compared to mammals, which exhibit more extreme chromosomal rearrangements [12,13,58,128,129,130,131,132], there are varying rates of change amongst phylogenetic groups. For example, passerine birds, being the most recently evolved avian order, display a greater rate of karyotypic evolution at the intrachromosomal (but not the interchromosomal) level and, at the same time, show a heightened speciation rate [131,133,134].
Early comparative genomics of avian karyotypes using classic banding techniques or FISH (see Section 2.1 above) indicated that bigger microchromosomes can, rarely, fuse by Robertsonian translocation [135] to form bi-armed macrochromosomes [11,12,23]. Centromeric locations can change from telocentric to bi-armed as a result of microchromosomes translocating preferentially to telocentric macrochromosomes (reviewed in [58]).

3.2. The Case of Chromosome 4

Through comparative cytogenetics, including G-banding and Zoo-FISH (using BAC clones and chromosome painting), it has been established that chicken chromosome 4 came into being as a fusion between ancestral chromosome 4 and a smaller chromosome in various bird species [12,25,136,137,138,139]. In guinea fowl (Numida meleagris, Galliformes), chromosome 4 arose as result of a centric fusion between chromosome 9 and the long (q) arm of the chicken chromosome 4 homolog [140]. This fusion involving the ancestral avian chromosome 4 is particularly significant, as the q arm of chicken chromosome 4 shows strong conservation to chromosome 4 in humans, indicating its presence in a common ancestor and suggesting about 310 million years of genomic stability [127,141,142]. Chromosome painting investigations (Zoo-FISH) revealed that several other avian species, such as the chicken, also demonstrate a fusion of the ancestral avian chromosomes 4 and 10, suggesting instances of possible homoplasy (convergence) [12]. In most other species examined, including all Palaeognathae species studied so far, the two chromosomes appear separate [13,143]. Furthermore, the short arm of chromosome 4 is homologous to an ancestral small chromosome, with Zoo-FISH data revealing interstitial telomeric signals adjacent to the centromere [12,23]. This ancestral region seems to have retained the characteristic microchromosomal traits of high recombination rate and density of genes. The recurring pattern of this rearrangement across various species might represent an instance of homoplasy, resulting from multiple independent fusions, or it could serve as an intriguing example of hemiplasy [13]. In Figure 1, the instances where convergence fusion of chromosome 4 with a microchromosome has been observed are denoted.
Gallus gallus chromosome-specific paints derived from chromosomes 1–9 and Z hybridized to metaphases of other Galliformes and Anseriformes revealed no further interchromosomal rearrangements [120,136,140,144]. Comparative mapping (by FISH) of selected chicken BAC clones also hybridized to chromosomes 1–8 and Z provided strong evidence for conservation between the sequences in the genomes of chicken, quail, turkey, and duck [29,145,146,147], representing very little change in two very early avian lineages (Galliformes and Anseriformes) that diverged nearly 90 MYA [137].

3.3. Rare Fusions of Microchromosomes in Selected Groups

The diploid (2n) chromosome counts in selected groups of birds, such as Ciconiiformes, Psittaciformes and Falconiformes, are lower [148,149,150] in stark contrast to the standard avian karyotype. Among these, the order Falconiformes (encompassing falcons and caracaras) has been particularly well studied [34,151]. Intensive cytogenetic analyses suggest that they possess the least typical chromosomal organization of all birds, characterized by an extremely low number of microchromosomes (typically one to six pairs). In contrast to most other birds therefore, the evolutionary rearrangements in Falconiformes favor the evolution of macrochromosomes rather than microchromosomes [13,15,132,151,152].
To enhance our understanding of significant genomic reorganizations in other birds of prey, de Oliveira et al. [153] focused on the harpy eagle (Harpia harpyja, Accipitriformes). Their study using chromosome painting revealed that this species lacks a clear distinction between micro- and macrochromosomes, with no apparent preference or restriction regarding this organization. Nanda et al. [152] applied chicken macrochromosome paints to metaphase preparations of three Old World vultures, which belong to different evolutionary clades within the Accipitridae family, to assess chromosomal conservation among these species. Their analysis uncovered extensive reshuffling of macrochromosomes among Old World vultures, a pattern that starkly differs from that observed in eagles.

3.4. A Classical Comparison Example: Chicken vs. Turkey vs. Zebra Finch

At a molecular, as well as the aforementioned cytogenetic, level, bird genomes are believed to have evolved at a slower pace compared to, e.g., mammals, making them suitable for successful cross-species hybridization using chromosome paints, BAC-based FISH, and OVERGO-based BAC library screenings [28,36,143,154,155]. One such classical example of avian comparative cytogenomic studies includes chicken, turkey and zebra finch that were the very first three bird species for which whole genome sequences were generated [16,156,157].
Chromosome painting investigations (chicken chromosomes 1–9 + Z) uncovered widespread homology between all three species, with the only difference being the aforementioned chromosome 4 scenario. The thorough comparative genomics of chicken and zebra finch [158] was made possible by the isolation of zebra finch BACs homologous to those in chicken and bioinformatic techniques (GenAlyzer tool [159]). Skinner and Griffin [134] employed bioinformatic strategies to map evolutionary cytogenomic differences between these three birds and provided an initial indication of the relative rate of intrachromosomal change in Passeriformes compared to other groups.
Preliminary studies on these species conducted by Romanov and Dodgson [28,160] included cross-species hybridizations making use of OVERGO probes derived from zebra finch Expressed Sequence Tags (ESTs) as well as chicken genomic data to interrogate BAC libraries of both zebra finch and turkey. As was anticipated, the success of hybridization was significantly greater for chicken–turkey experiments compared to zebra finch combined with either of the other two, especially for OVERGOs found within coding sequences as opposed to within introns, flanking sequences or untranslated regions. This made the “one sequence, multiple genomes” approach easier. An extensive set of orthologous data points that correspond to BACs connected to the genes of chickens, turkeys, and zebra finches via interspecies hybridization was made accessible online [28,43]. Moreover, the success rates of comparative genomics by physical mapping alongside other avian genomes using pan-species OVERGO–BAC hybridization fit well with their divergence during evolution [28,36,40,161].

3.5. Emu, Ostrich and One Extinct Species

The emu is a palaeognathous ratite bird, and the only extant member of the Dromaiini tribe that, alongside cassowaries, falls under the order Casuariiformes [58,162]. Emus and cassowaries share a common ancestor from the Pliocene epoch (5–10 MYA) [58,162]. Found in open woodlands and semi-arid regions of Australia and Tasmania, emus have been successfully bred in captivity primarily for their meat since the 1970s, contributing to a national flock that exceeded 30,000 birds by 1994. Their popularity is increasing due to markets for their meat, feathers, oil and hide [163]. The ostrich—the world’s largest bird and the only extant representative of the family Struthionidae—attracts much genomic interest largely because of funding derived from its agricultural value as a source of meat. Both the emu and the ostrich’s karyotype consist of 2n = 80 chromosomes. Some of the very earliest work involving Zoo-FISH was performed on these species [25,164].
The emu has a high-quality draft genome assembly complemented by extensive long-read sequencing data [165] and has one of the most completely assembled genomes among the ratites [166]. Liu et al. [165] established that the centromeres of the small emu microchromosomes (which are gene-rich) cluster at the nuclear center, away from the macrochromosomes, which are located at the periphery and show several interchromosomal connections between housekeeping genes. Unlike non-ratite birds, regions of chromosome W of the emu have diverged between the sexes and lost homologous recombination in less than one-third of its length. WS0, a highly heterochromatic region, and WS1, a more recently formed area with only slight sequence divergence from the Z chromosome, make up the two portions of the W chromosome. Heterochromatin from WS0 appears to have enlarged its inactive chromatin compartment, enhanced chromatin contacts inside WS1, and decreased interactions with adjacent regions. These observations have led to suggestions that chromatin conformation changes play a key role early in the evolution of sex chromosomes [165]. Moreover, use of Hi-C technology (e.g., [167]) has revealed high-order chromatin folding as a primary driver of gene co-regulation across the avian tree of life. Specifically, condensin II has been discovered to be a determinant of architecture type [168], and three-dimensional remodeling of the avian germ line has a significant role in modulating evolutionary plasticity [169].
Similarly, the ostrich has a well-described genome assembly supplemented by optical mapping studies [95]. The genome size is comparatively large (~1.25 Gb) consistent with other ratite birds studied. The similarity in overall karyotype/genome organization of chicken, turkey, zebra finch, ostrich and emu provided strong evidence that they all had a genome organization that resembled an avian protokaryotype, from which all others were derived.
Emu and ostrich are both examples of ratite birds from the Palaeognathae. While most of our conclusions about ancient DNA are based on extrapolations, at least one species, the little bush moa (ratite paleognath Anomalopteryx didiformis, Dinornithiformes), has had a partial genome sequence assembly performed [170]. Successful reconstructions of ancient DNA largely depend on the age of the specimen and the conditions in which it was preserved.

3.6. Cytogenomics of the California Condor

The California condor is an endangered bird species historically classified within the order Ciconiiformes (storks), specifically in the family Cathartidae, which includes New World vultures [171]. It was one of the first New World birds in which detailed cytogenomic studies were performed [40,67,138]. The classification of cathartids has been contentious, as earlier studies placed this group alongside Old World vultures in the order Falconiformes [172]. A preliminary investigation utilizing 5000 bp sequences from five nuclear genes and innovative phylogenetic methods proposed elevating New World vultures to a distinct order that is more closely related to Falconiformes than to a clade comprising storks and related birds [173]. Currently, Cathartidae is well established as the singular family within the separate order Cathartiformes [1,174]. California condors are among the largest flying birds in North America, with wingspans reaching 9–10 feet. They played a vital ecological role across a broad range that included the western and southern USA and Mexico, acting as nature’s scavengers. These birds can cover 150 miles per day in search of carrion, achieve speeds of up to 55 mph, soar to heights of 15,000 ft, and can last several days without food [40,65,175].
To advance the genomic analysis of this endangered species and leverage developments in chicken genomics, a comprehensive cytogenetic study by Raudsepp et al. [138] identified a total diploid chromosome number of 2n = 80 (potentially with an extra pair of microchromosomes). Identifying similarities to the ancestral avian karyotype, these studies provided insights into the locations of nucleolar organizing regions, telomeres and centromeres [138]. A comparative map comparing condor and chicken macrochromosomes was also constructed using individual chicken chromosome-specific paints for chicken chromosomes 1–9 + ZW on condor chromosome spreads. Each chicken macrochromosome, except for chromosomes 4 and Z, corresponded to a single condor macrochromosome. Notably, the chromosome 4 paint revealed homology with two California condor chromosomes, 4 and 9, further supporting the notion that these latter chromosomes are ancestral to avian species and chicken chromosome 4 is a rare fusion. The Z chromosome paint hybridized to both sex chromosomes (Z and W) in the condor, indicating that the condor’s sex chromosomes are not fully differentiated compared to those in other non-ratite birds [138].
A large-insert BAC library of the California condor was developed at the BACPAC Center [40], yielding ~14× coverage of this bird’s genome. Making use of this library, a first-generation comparative physical map between this species and the chicken was established via an OVERGO hybridization approach [40]. This comparison indicated a high degree of synteny conserved between the two birds’ genomes, as demonstrated by aligning specific condor BAC sequences with their chicken orthologs. Subsequently, the BAC-based comparative map of chicken and condor was updated, containing 192 loci that were anchored to California condor BACs that were derived from the sequences of several bird species, including (as well as chicken and condor) zebra finch and other New World vultures [65]. This effort also facilitated the identification and characterization of candidate loci associated with a chondrodystrophy mutation in California condors, furthering the genetic management of this condition [64,66,71]. Among ~200 genes identified in the condor BAC library, numerous functional candidate genes that are involved in the development of cartilage and bone were located, including aggrecan 1 (AGC1). This gene has been demonstrated to contribute to skeletal dysplasia in a number of model birds (chicken, turkey, Japanese quail) and mammals (mouse and human) [176,177].
Subsequently, to assess the applicability of the condor BAC library for cross-species hybridization and to develop the California condor cytogenetic map, a FISH study was conducted using ~70 BACs from both California condor and chicken [154]. Most of the BACs mapped to condor chromosomes were homologous to corresponding chicken genes and chromosomes, confirming a substantial degree of conserved synteny between the two genomes. An intrachromosomal rearrangement was detected on chromosome 4, along with additional rearrangements identified on the Z chromosome. In some instances, a clone corresponding to a Z-linked gene was found mapped to an autosome [154]. Further FISH analyses are warranted in the California condor to verify these inter- and intrachromosomal rearrangements.
Through the sequencing of clones from a California condor microsatellite-enriched library [65], a total of 951 short genomic sequences were isolated, with approximately 30% found to be homologous to avian sequences, including nearly all the chicken chromosomes during in silico mapping. Many of these sequences encompassed microsatellites and other repetitive elements, such as CR1, various long interspersed nuclear elements (LINEs), retroviral LTRs and satellites that are recognized in chickens [65]. Interestingly, tandemly repeated HaeIII satellite DNA sequences, previously identified only in other New World vultures [178], were also detected in the California condor. A first-generation genetic linkage map for condors has been produced [171], and parentage analysis in condors using the established polymorphic microsatellite loci identified two cases of parthenogenetic reproduction [179]. Additionally, a total of 13 BACs homologous to human chromosome number 7 and six chromosomes from chicken have been sequenced in collaboration with the National Institutes of Health (NIH). This resulted in a comparative physical map for a region corresponding to human chromosome 7 that is accessible online through the NIH database [65].
In partnership with the Washington University Genome Sequencing Center, ~440,000 cDNA sequences were isolated from a Californian condor fibroblast cell line using cutting-edge 454 technology and subsequently deposited in the National Center for Biotechnology Information (NCBI) Trace Archive. These data provided an initial glimpse into the condor transcriptome, facilitating future research in California condor genomics and comparative avian genomics [65]. Ultimately, a high-quality, chromosome-length assembly of the California condor genome was produced, and its genome-wide diversity was explored [67,180,181]. Comparative genomic experiments were also carried out on the genomes of two closely related species—the turkey vulture (Cathartes aura, Accipitriformes) and the Andean condor (Vultur gryphus, Accipitriformes). Evidence of historical population declines was found in the genomes of all three species. Remarkably, the California condor’s genome retains a significant amount of diversity, reflecting its historically higher population numbers. Additionally, a history of purifying selection against linked deleterious alleles was suggested by correlations between genome-wide diversity and recombination rates, indicating promising prospects for future conservation efforts [180].

3.7. Bald Eagle

This iconic North American bird of prey (Haliaeetus leucocephalus, Accipitriformes), known as the national bird of the United States, belongs to the family Accipitridae and the order Accipitriformes [182,183]. While the bald eagle is classified as threatened in southern Canada and much of the USA, it remains abundant in its northern habitats, particularly Alaska [184]. Its karyotype comprises 2n = 66 chromosomes, including as little as four pairs of microchromosomes, with tiny satellites present on the fourth largest chromosomal pair [185]. The genomic data for the bald eagle were generated as part of the Avian Phylogenomic Project [186], yielding 1.26 Gb of high-quality sequencing scaffolds with a contig and scaffold N50 of 10 Kb and 670 Kb, respectively. The analysis identified a total of 16,526 protein-coding genes with an average length of 19 Kb [187]. Judkins et al. [188] generated data through restriction-site-associated DNA (RAD)-tag and low-coverage resequencing of the whole genome. These were mapped to the bald eagle reference genome [187] to create a 50K single-nucleotide polymorphism (SNP) array that helped reveal the genetic structure of bald eagles [188].

3.8. Falconiformes

In Falconiformes (falcons and relatives), significant rearrangements have occurred, with the regions homologous to microchromosomes 10, 12, 13, 14, 15, 17, 18, 19, 20, 21, 23, and 28 in chicken fused to regions of chicken macrochromosomes in gyr, saker and peregrine falcons (Falco rustcolus, F. cherrug and F. peregrinus, respectively) [34,151]. Lineage-specific rearrangements were evident, as there was no indication of rearrangements for homologs of chicken chromosomes 15, 18, 19, 23, and 28 in any of the other tested (non-falcon-related) species. Notably, chromosomes 15, 18, and 19 have merged into a single chromosome comparable to chicken homolog 4 in all falcon species examined. Chromosomes 23 and 28 have also fused to the homolog of chicken chromosome 2, which appears to have split into two chromosomes at some point, either before or after their fusion. All falcon species tested (peregrine, gyr and saker) displayed the same rearrangement pattern, with the exception of peregrine chromosome 1, which showed a centric fusion [34]. This suggests that any lineage-specific rearrangements quickly became established within the population with minimal interchromosomal rearrangement since then. Moreover, there seems to be no interchromosomal rearrangement between each pair of tested BACs, indicating that these DNA regions are highly conserved and resistant to breakage [34].

3.9. Indian Roller

This bird (Coracias benghalensis), found across tropical southern Asia from Iraq to Thailand, belongs to the Coraciidae family in the order Coraciiformes [189]. Although it occasionally travels, it is not migratory. Its karyotype has distinct characteristics, featuring a diploid number of approximately 2n = 88, with as little as two pairs of large macrochromosomes, a medium-sized Z chromosome, plus a small W chromosome; all other chromosomes are microchromosomes or dot chromosomes [190]. The species was included in a study with the aim of examining the evolutionary relationships between 16 Coraciidae birds through genomic sequences generated from a total of 15 nuclear genes and their total mitochondrial genomes [189]. The subspecies C. benghalensis affinis from Southeast Asia is clustered with the purple-winged roller (C. temminickii) from Sulawesi, and forms a sister group with C. benghalensis benghalensis from India and Western Asia. More recently, the genome sequencing of the Indian roller was published, but further public data has not yet been released at the time of writing [191].

3.10. Psittaciformes

Within Psittaciformes, four species have been studied using microchromosome BAC probes: the kakariki (Cyanoramphus novaezelandiae), the cockatiel (Nymphicus hollandicus), the budgerigar (Melopsittacus undulatus), and the monk parakeet (Myiopsitta monachus) [33,34,150,192]. While these initial physical mappings suggested an absence of sex chromosome rearrangements [150], recent chromosome-level genome assemblies have refined this understanding. It is now evident that a fusion between microchromosome 11 and the ancestral Z chromosome occurred in the common ancestor of parrots, creating a neo-sex chromosome system shared across the order [193]. Moreover, in the monk parakeet, a second fusion event involving microchromosome 25 was identified. Although this rearrangement was previously interpreted as an autosomal fusion involving chromosome 4, genomic data confirmed its integration into the neo-Z chromosome. These successive fusions, along with extensive macro- and microchromosome reshuffling, have resulted in the reduced diploid number of 2n = 48 observed in this species [150,193].

3.11. Pelecaniformes

Molecular cytogenetics in this order remains limited, although recent investigations using chromosome painting strategies with chicken and/or Eurasian stone curlew (Burhinus oedicnemus) paints have demonstrated that the karyotype of Pelecaniformes is reorganized [148]. Chromosome painting using stone curlew data in three Pelecaniformes species—Ardea cinerea (grey heron), Egretta garzetta (little egret), and Nipponia nippon (crested ibis)—established that individual lineages within Pelecaniformes display distinct chromosomal rearrangements [148,194]. The primary changes observed were fusion events involving both the macro- and microchromosomes [148]. For instance, in the whistling heron (Syrigma sibilatrix), the chicken paints from chromosomes 8, 9, and 10 hybridized to the long (q) arms of bi-armed macrochromosomes, indicating fusions with microchromosomes. While B. oedicnemus and chicken microchromosome paints do not facilitate identification of the specific microchromosomes involved in these fusion events, these findings nonetheless suggest that such fusions are common among Pelecaniformes (reviewed in [13]). Furthermore, in N. nippon, it has been specifically identified that microchromosome 22 has fused to the W and Z sex chromosomes, originating a neo-Z and neo-W system [195].

3.12. Ciconiiformes

Most studies on the chromosome organization of storks (Ciconiiformes) have primarily utilized conventional staining methods [196,197]. Notwithstanding, an interesting variation in diploid chromosome numbers has been noted, ranging from 2n = 52 to 78. Given that many species exhibit similar macrochromosomes, some researchers suggest that karyotype evolution mainly results from fusions involving microchromosomes, a hypothesis later supported by chromosome painting. However, the specific microchromosomes involved in these rearrangements have not yet been identified, indicating a need for further research (reviewed in [13]).

3.13. Caprimulgiformes, Cuculiformes, Suliformes, Sphenisciformes, and Passeriformes

Most Passeriformes and Caprimulgiformes species display the typical avian karyotype [14], as demonstrated through microchromosomal BAC FISH analysis, with only one species, yellow-olive flatbill (Tolmomyias sulphurescens, 2n = 60, Rhynchocyclidae, Passeriformes), out of seven studied exhibiting microchromosomal fusions [198]. This low diploid number likely pertains specifically to the Rhynchocyclidae family, while remaining conserved in other passeriform species (reviewed in [13]).

4. Sex Chromosomal Changes

As mentioned in Section 2.9, the avian genome and its associated karyotype is characterized by a ZZ/ZW system. For most birds, apart from the ratites, the sex chromosomes are distinguishable from one another in females. Recent Zoo-FISH studies have, however, revealed unexpected degree of dynamism in bird sex chromosomes, challenging previous notions of their stability [193,199,200]. That is, although the Z chromosome was thought to be relatively stable evolutionarily [201], recent work [193,199,200,202] is uncovering high rates of intrachromosomal rearrangement in certain species. The first multiple sex-chromosome system in birds was discovered in the Adélie penguin (Pygoscelis adeliae, Sphenisciformes), where males exhibit 2n = 96 and females 2n = 95. This system originated from a fusion between a microchromosome and the W chromosome in the species’ ancestor [203]. This multiple sex-chromosome system can be defined as follows: ♂Z1Z1Z2Z2/♀Z1Z2W [203]. Additionally, genomic investigations uncovered instances of independent fusion events between autosomes and sex chromosomes in Sylvioidea species [204]. Neo-sex chromosomes have also been detected in parrots [193], with similar discoveries reported in certain cuckoo species [199,200]. These findings collectively underscore a previously unidentified dynamism and diversity pertaining to avian sex chromosomes.
Subsequently, within Suliformes, the genus Sula (boobies) was also described as having a multiple sex-chromosome system; males exhibit 2n = 76 (Z1Z1Z2Z2), while females show 2n = 75 (Z1Z2W). This system similarly arose from an uncharacterized microchromosome–W fusion in the ancestor of extant Sula species [205]. Within Cuculiformes, the smooth-billed ani (Crotophaga ani) is the only species studied to date using BAC–FISH. This analysis revealed extensive chromosomal reorganization involving both macro- and microchromosomes, including a fusion between the ancestral chicken chromosome 17 (GGA17) and the Z chromosome [200]. Further testing in the guira cuckoo (Guira guira) confirmed that this GGA17–Z fusion is also present in that species [199].
Autosome-to-Z chromosome Robertsonian translocations remain rare in birds, having been observed primarily in Sylvioidea species (Passeriformes) involving chromosomes 3, 4, 4a and 5 [204]. Similar rearrangements occur within the Meliphagidae family (Passeriformes), specifically in the blue-faced honeyeater (Entomyzon cyanotis), sooty myzomela (Myzomela tristrami), and cardinal myzomela (M. cardinalis), where the Z chromosome has fused with chromosome 5 [206,207]. Additionally, these translocations have been identified in selected parrot species through genome sequencing, as synthesized in recent reviews (e.g., [13]). Instances of sex chromosomes being fused to autosomes (and hence forming neo-sex chromosomes) are illustrated on the right-hand side of Figure 1.

5. Conclusions

Overall, the typical avian karyotype, by and large as epitomized by the chicken, is a mode of genome organization laid down before the emergence of the dinosaurs (245 MYA) and persisting to the present day [208]. When the first chromosome preparations of birds were made, a reasonable assumption would have been that the high diploid number and preponderance of microchromosomes underpinned a rapidly changing and highly dynamic environment. In fact, the opposite proved to be the case: karyotypes were quite similar to one another. More detailed chromosome painting experiments (Zoo-FISH) similarly revealed very few interchromosomal rearrangements, and even fewer changes were observed in the microchromosomes when cross-species BACs were employed. In fact, the more we looked, the more we found similarities than differences—a situation in stark contrast to that of studying mammals, where interspecific chromosomal changes were commonplace. In a moment of rare fortuity, it turned out that the species that had been the most studied—chicken (popular because of its relevance to food production and developmental biology, amongst other things)—had the karyotype most like that of the avian ancestor. Rare, derived changes such as the fusion of chromosome 4 to a microchromosome did not detract from the fact that chicken could be used as a genomic model of all birds. Contrast this to the situation in mammals, where the most studied non-human mammalian model in genetics, the mouse, had an inordinate number of genomic rearrangements compared to other species. In the background of very little chromosomal change therefore, it could be argued that, when changes do occur, they are more likely to be biologically meaningful. Through the study of bird karyotype evolution, therefore, we might gain a greater insight into the functional reasons for chromosomal change.

Author Contributions

Conceptualization, M.N.R., R.K., D.M.L. and D.K.G.; validation, L.C.P., K.S., R.E.O., R.K., M.N.R. and D.K.G.; formal analysis, L.C.P., R.K., M.N.R. and D.K.G.; investigation, R.K., M.N.R. and D.K.G.; data curation, R.K., M.N.R. and D.K.G.; writing—original draft preparation, M.N.R., R.K. and D.K.G.; writing—review and editing, D.M.L., R.E.O., R.K., K.S., W.S., M.N.R. and D.K.G.; visualization, D.K.G., L.C.P., R.K. and M.N.R.; supervision, D.K.G.; project administration, D.K.G. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Institutional Review Board Statement

The biological material was obtained following permission from Sistema de Autorização e Informação em Biodiversidade approved in 30 September 2020 (SISBIO 61047-3) and the ethics committee of Universidade Federal do Pampa approved in 30 November 2020 (019/2020).

Informed Consent Statement

Not applicable.

Data Availability Statement

No new data were created or analyzed in this study. Data sharing is not applicable to this article.

Conflicts of Interest

The authors declare no conflicts of interest.

Abbreviations

The following abbreviations are used in this manuscript:
2nchromosome diploid number
AGC1aggrecan 1
BACbacterial artificial chromosome
DMRT1doublesex and mab-3-related transcription factor 1
FERFER tyrosine kinase
FISHfluorescence (or fluorescent) in situ hybridization
Gbgigabase (1 billion (109) base pairs)
GGA1chicken (Gallus gallus) chromosome 1
GGA17chicken (Gallus gallus) chromosome 17
GGA20chicken (Gallus gallus) chromosome 20
GGA26chicken (Gallus gallus) chromosome 26
GHRgrowth hormone receptor
HiFisingle-molecule, high-fidelity sequencing
IGF2BP1insulin-like growth factor 2 mRNA binding protein 1
K–PgCretaceous–Paleogene boundary
LAL20white hawk (Leucopternis albicollis) chromosome 20
LTRlong terminal repeat retrotransposon
Mbmegabase (1 million (106) base pairs)
MITFmelanocyte-inducing transcription factor
MYAmillion years ago
NDPnorrin cystine knot growth factor NDP
RADrestriction-site-associated DNA
SMRTsingle-molecule, real-time sequencing
SNPsingle-nucleotide polymorphism
SRYsex-determining region Y
TEstransposable elements
XXhomogametic females in mammals
XYmammalian sex chromosome system, also heterogametic males in mammals
ZWavian sex chromosome system, also heterogametic females in birds
ZZhomogametic males in birds

References

  1. Jarvis, E.D.; Mirarab, S.; Aberer, A.J.; Li, B.; Houde, P.; Li, C.; Ho, S.Y.W.; Faircloth, B.C.; Nabholz, B.; Howard, J.T.; et al. Whole-genome analyses resolve early branches in the tree of life of modern birds. Science 2014, 346, 1320–1331. [Google Scholar] [CrossRef] [Scilit]
  2. Stiller, J.; Feng, S.; Chowdhury, A.-A.; Rivas-González, I.; Duchêne, D.A.; Fang, Q.; Deng, Y.; Kozlov, A.; Stamatakis, A.; Claramunt, S.; et al. Complexity of avian evolution revealed by family-level genomes. Nature 2024, 629, 851–860. [Google Scholar] [CrossRef] [Scilit]
  3. AviList Core Team. AviList: The Global Avian Checklist, v2025. 2025. Available online: https://www.avilist.org/checklist/v2025/ (accessed on 17 May 2026).
  4. Fänger, H. Avitaxonomicon Website. 2024. Available online: https://www.bird-phylogeny.de (accessed on 17 May 2026).
  5. Braun, E.L.; Kimball, R.T. Data types and the phylogeny of Neoaves. Birds 2021, 2, 1–22. [Google Scholar] [CrossRef] [Scilit]
  6. Cloutier, A.; Sackton, T.B.; Grayson, P.; Clamp, M.; Baker, A.J.; Edwards, S.V. Whole-genome analyses resolve the phylogeny of flightless birds (Palaeognathae) in the presence of an empirical anomaly zone. Syst. Biol. 2019, 68, 937–955. [Google Scholar] [CrossRef] [Scilit]
  7. Berv, J.S.; Field, D.J. Genomic signature of an avian Lilliput effect across the K-Pg extinction. Syst. Biol. 2018, 67, 1–13. [Google Scholar] [CrossRef] [Scilit]
  8. Berv, J.S.; Singhal, S.; Field, D.J.; Walker-Hale, N.; McHugh, S.W.; Shipley, J.R.; Miller, E.T.; Kimball, R.T.; Braun, E.L.; Dornburg, A.; et al. Genome and life-history evolution link bird diversification to the end-Cretaceous mass extinction. Sci. Adv. 2024, 10, eadp0114. [Google Scholar] [CrossRef] [Scilit]
  9. Schulte, P.; Alegret, L.; Arenillas, I.; Arz, J.A.; Barton, P.J.; Bown, P.R.; Bralower, T.J.; Christeson, G.L.; Claeys, P.; Cockell, C.S.; et al. The Chicxulub asteroid impact and mass extinction at the Cretaceous-Paleogene boundary. Science 2010, 327, 1214–1218. [Google Scholar] [CrossRef] [Scilit]
  10. Kiazim, L.G.; O’Connor, R.E.; Larkin, D.M.; Romanov, M.N.; Narushin, V.G.; Brazhnik, E.A.; Griffin, D.K. Comparative mapping of the macrochromosomes of eight avian species provides further insight into their phylogenetic relationships and avian karyotype evolution. Cells 2021, 10, 362. [Google Scholar] [CrossRef] [Scilit]
  11. Christidis, L. Aves. In Animal Cytogenetics. Volume 4: Chordata 3 B; John, B., Kayano, H., Levan, A., Eds.; Gebrüder Borntraeger: Berlin, Germany, 1990. [Google Scholar]
  12. Griffin, D.K.; Robertson, L.B.W.; Tempest, H.G.; Skinner, B.M. The evolution of the avian genome as revealed by comparative molecular cytogenetics. Cytogenet. Genome Res. 2007, 117, 64–77. [Google Scholar] [CrossRef] [Scilit]
  13. O’Connor, R.E.; Kretschmer, R.; Romanov, M.N.; Griffin, D.K. A bird’s-eye view of chromosomic evolution in the Class Aves. Cells 2024, 13, 310. [Google Scholar] [CrossRef] [Scilit]
  14. Degrandi, T.M.; Barcellos, S.A.; Costa, A.L.; Garnero, A.d.V.; Hass, I.; Gunski, R.J. Introducing the bird chromosome database: An overview of cytogenetic studies in birds. Cytogenet. Genome Res. 2020, 160, 199–205. [Google Scholar] [CrossRef] [Scilit]
  15. Huang, Z.; Xu, Z.; Bai, H.; Huang, Y.; Kang, N.; Ding, X.; Liu, J.; Luo, H.; Yang, C.; Chen, W.; et al. Evolutionary analysis of a complete chicken genome. Proc. Natl. Acad. Sci. USA 2023, 120, e2216641120. [Google Scholar] [CrossRef] [Scilit]
  16. International Chicken Genome Sequencing Consortium. Sequence and comparative analysis of the chicken genome provide unique perspectives on vertebrate evolution. Nature 2004, 432, 695–716. [Google Scholar] [CrossRef] [Scilit]
  17. Romanov, M.N.; Farré, M.; Lithgow, P.E.; Fowler, K.E.; Skinner, B.M.; O’Connor, R.; Fonseka, G.; Backström, N.; Matsuda, Y.; Nishida, C.; et al. Reconstruction of gross avian genome structure, organization and evolution suggests that the chicken lineage most closely resembles the dinosaur avian ancestor. BMC Genom. 2014, 15, 1060. [Google Scholar] [CrossRef] [Scilit]
  18. McQueen, H.A.; Siriaco, G.; Bird, A.P. Chicken microchromosomes are hyperacetylated, early replicating, and gene rich. Genome Res. 1998, 8, 621–630. [Google Scholar] [CrossRef] [Scilit]
  19. Smith, J.; Paton, I.R.; Bruley, C.K.; Windsor, D.; Burt, D.W.; Ponce de Leon, F.A.; Burke, D. Integration of the genetic and physical maps of the chicken macrochromosomes. Anim. Genet. 2000, 31, 20–27. [Google Scholar] [CrossRef] [Scilit]
  20. Habermann, F.A.; Cremer, M.; Walter, J.; Kreth, G.; Von Hase, J.; Bauer, K.; Wienberg, J.; Cremer, C.; Cremer, T.; Solovei, I. Arrangements of macro- and microchromosomes in chicken cells. Chromosome Res. 2001, 9, 569–584. [Google Scholar] [CrossRef] [Scilit]
  21. Burt, D.W. Origin and evolution of avian microchromosomes. Cytogenet. Genome Res. 2002, 96, 97–112. [Google Scholar] [CrossRef] [Scilit]
  22. Masabanda, J.S.; Burt, D.W.; O’Brien, P.C.M.; Vignal, A.; Fillon, V.; Walsh, P.S.; Cox, H.; Tempest, H.G.; Smith, J.; Habermann, F.; et al. Molecular cytogenetic definition of the chicken genome: The first complete avian karyotype. Genetics 2004, 166, 1367–1373. [Google Scholar] [CrossRef] [Scilit]
  23. Griffin, D.K.; Haberman, F.; Masabanda, J.; O’Brien, P.; Bagga, M.; Sazanov, A.; Smith, J.; Burt, D.W.; Ferguson-Smith, M.; Wienberg, J. Micro- and macrochromosome paints generated by flow cytometry and microdissection: Tools for mapping the chicken genome. Cytogenet. Genome Res. 1999, 87, 278–281. [Google Scholar] [CrossRef] [Scilit]
  24. Wienberg, J.; Jauch, A.; Stanyon, R.; Cremer, T. Molecular cytotaxonomy of primates by chromosomal in situ suppression hybridization. Genomics 1990, 8, 347–350. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  25. Shetty, S.; Griffin, D.K.; Graves, J.A.M. Comparative painting reveals strong chromosome homology over 80 million years of bird evolution. Chromosome Res. 1999, 7, 289–295. [Google Scholar] [CrossRef] [Scilit]
  26. Langer-Safer, P.R.; Levine, M.; Ward, D.C. Immunological method for mapping genes on Drosophila polytene chromosomes. Proc. Natl. Acad. Sci. USA 1982, 79, 4381–4385. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Lithgow, P.E.; O’Connor, R.; Smith, D.; Fonseka, G.; Rathje, C.; Frodsham, R.; O’Brien, P.C.; Ferguson-Smith, M.A.; Skinner, B.M.; Griffin, D.K.; et al. Novel Tools for Characterising Inter- and Intra-chromosomal Rearrangements in Avian Microchromosomes. In Proceedings of the 2014 Meeting on Avian Model Systems, Cold Spring Harbor, NY, USA, 5–8 March 2014; Cold Spring Harbor Laboratory: Cold Spring Harbor, NY, USA, 2014; p. 56. Available online: https://kar.kent.ac.uk/46692/ (accessed on 17 May 2026).
  28. Romanov, M.N.; Dodgson, J.B. Cross-species overgo hybridization and comparative physical mapping within avian genomes. Anim. Genet. 2006, 37, 397–399. [Google Scholar] [CrossRef] [Scilit]
  29. Griffin, D.K.; Robertson, L.B.; Tempest, H.G.; Vignal, A.; Fillon, V.; Crooijmans, R.P.; Groenen, M.A.; Deryusheva, S.; Gaginskaya, E.; Carré, W.; et al. Whole genome comparative studies between chicken and turkey and their implications for avian genome evolution. BMC Genom. 2008, 9, 168. [Google Scholar] [CrossRef] [Scilit]
  30. Skinner, B.M.; Robertson, L.B.; Tempest, H.G.; Langley, E.J.; Ioannou, D.; Fowler, K.E.; Crooijmans, R.P.; Hall, A.D.; Griffin, D.K.; Völker, M. Comparative genomics in chicken and Pekin duck using FISH mapping and microarray analysis. BMC Genom. 2009, 10, 357. [Google Scholar] [CrossRef] [Scilit]
  31. Damas, J.; O’Connor, R.; Farré, M.; Lenis, V.P.E.; Martell, H.J.; Mandawala, A.; Fowler, K.; Joseph, S.; Swain, M.T.; Griffin, D.K.; et al. Upgrading short-read animal genome assemblies to chromosome level using comparative genomics and a universal probe set. Genome Res. 2017, 27, 875–884. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. O’Connor, R.E.; Romanov, M.N.; Kiazim, L.G.; Barrett, P.M.; Farré, M.; Damas, J.; Ferguson-Smith, M.; Valenzuela, N.; Larkin, D.M.; Griffin, D.K. Reconstruction of the diapsid ancestral genome permits chromosome evolution tracing in avian and non-avian dinosaurs. Nat. Commun. 2018, 9, 1883. [Google Scholar] [CrossRef] [Scilit]
  33. O’Connor, R.E.; Kiazim, L.; Skinner, B.; Fonseka, G.; Joseph, S.; Jennings, R.; Larkin, D.M.; Griffin, D.K. Patterns of microchromosome organization remain highly conserved throughout avian evolution. Chromosoma 2019, 128, 21–29. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. O’Connor, R.E.; Farré, M.; Joseph, S.; Damas, J.; Kiazim, L.; Jennings, R.; Bennett, S.; Slack, E.A.; Allanson, E.; Larkin, D.M.; et al. Chromosome-level assembly reveals extensive rearrangement in saker falcon and budgerigar, but not ostrich, genomes. Genome Biol. 2018, 19, 171. [Google Scholar] [CrossRef] [Scilit]
  35. Sazanov, A.A.; Romanov, M.N.; Sazanova, A.L.; Stekol’nikova, V.A.; Kozyreva, A.A.; Malewski, T.; Smirnov, A.F. Chromosomal localization of 15 HSA3p14–p21 NotI clones on GGA12: Orthology of a chicken microchromosome to a gene-rich region of HSA3. Anim. Genet. 2005, 36, 71–73. [Google Scholar] [CrossRef] [Scilit]
  36. Romanov, M.N.; Dodgson, J.B.; Gonser, R.A.; Tuttle, E.M. Comparative BAC-based mapping in the white-throated sparrow, a novel behavioral genomics model, using interspecies overgo hybridization. BMC Res. Notes 2011, 4, 211. [Google Scholar] [CrossRef] [Scilit]
  37. Romanov, M.N.; Griffin, D.K. The use of avian BAC libraries and clones. Cytogenet. Genome Res. 2015, 145, 94–96. [Google Scholar] [CrossRef] [Scilit]
  38. Clayton, D.F. Songbird genomics: Methods, mechanisms, opportunities, and pitfalls. Ann. N. Y. Acad. Sci. 2004, 1016, 45–60. [Google Scholar] [CrossRef] [Scilit]
  39. Kellner, W.A.; Sullivan, R.T.; Carlson, B.H.; Thomas, J.W. Uprobe: A genome-wide universal probe resource for comparative physical mapping in vertebrates. Genome Res. 2005, 15, 166–173. [Google Scholar] [CrossRef] [Scilit]
  40. Romanov, M.N.; Koriabine, M.; Nefedov, M.; de Jong, P.J.; Ryder, O.A. Construction of a California condor BAC library and first-generation chicken–condor comparative physical map as an endangered species conservation genomics resource. Genomics 2006, 88, 711–718. [Google Scholar] [CrossRef] [Scilit]
  41. Madishetty, K.; Condamine, P.; Svensson, J.T.; Rodriguez, E.; Close, T.J. An improved method to identify BAC clones using pooled overgos. Nucleic Acids Res. 2007, 35, e5. [Google Scholar] [CrossRef] [Scilit]
  42. Dodgson, J.B.; Romanov, M.N.; Rondelli, C.M. Integration of Chicken Linkage and Physical Maps and Sequence Alignment Using Overgo Hybridization. In Proceedings of the International Plant and Animal Genome XII Conference, San Diego, CA, USA, 10–14 January 2004; Abstract W215; Scherago International: San Diego, CA, USA, 2004; p. 59. Available online: https://kar.kent.ac.uk/46432/ (accessed on 17 May 2026).
  43. Romanov, M.N.; Price, J.A.; Dodgson, J.B. Integration of animal linkage and BAC contig maps using overgo hybridization. Cytogenet. Genome Res. 2003, 102, 277–281. [Google Scholar] [CrossRef] [Scilit]
  44. Song, B.-K.; Nadarajah, K.; Romanov, M.N.; Ratnam, W. Cross-species bacterial artificial chromosome (BAC) library screening via overgo-based hybridization and BAC-contig mapping of a yield enhancement quantitative trait locus (QTL) yld1.1 in the Malaysian wild rice Oryza rufipogon. Cell. Mol. Biol. Lett. 2005, 10, 425–437. [Google Scholar]
  45. Thomas, J.W.; Prasad, A.B.; Summers, T.J.; Lee-Lin, S.-Q.; Maduro, V.V.B.; Idol, J.R.; Ryan, J.F.; Thomas, P.J.; McDowell, J.C.; Green, E.D. Parallel construction of orthologous sequence-ready clone contig maps in multiple species. Genome Res. 2002, 12, 1277–1285. [Google Scholar] [CrossRef] [Scilit]
  46. Sullivan, R.T.; Morehouse, C.B.; NISC Comparative Sequencing Program; Thomas, J.W. Uprobe 2008: An online resource for universal overgo hybridization-based probe retrieval and design. Nucleic Acids Res. 2008, 36, W149–W153. [Google Scholar] [CrossRef] [Scilit]
  47. Meyer, A.; Zardoya, R. Recent advances in the (molecular) phylogeny of vertebrates. Annu. Rev. Ecol. Evol. Syst. 2003, 34, 311–338. [Google Scholar] [CrossRef] [Scilit]
  48. Prasad, A.B.; Allard, M.W.; Green, E.D.; NISC Comparative Sequencing Program. Confirming the phylogeny of mammals by use of large comparative sequence data sets. Mol. Biol. Evol. 2008, 25, 1795–1808. [Google Scholar] [CrossRef] [Scilit]
  49. Chen, K.; Wallis, J.W.; McLellan, M.D.; Larson, D.E.; Kalicki, J.M.; Pohl, C.S.; McGrath, S.D.; Wendl, M.C.; Zhang, Q.; Locke, D.P.; et al. BreakDancer: An algorithm for high-resolution mapping of genomic structural variation. Nat. Methods 2009, 6, 677–681. [Google Scholar] [CrossRef] [Scilit]
  50. Eisfeldt, J.; Pettersson, M.; Vezzi, F.; Wincent, J.; Käller, M.; Gruselius, J.; Nilsson, D.; Syk Lundberg, E.; Carvalho, C.M.; Lindstrand, A. Comprehensive structural variation genome map of individuals carrying complex chromosomal rearrangements. PLoS Genet. 2019, 15, e1007858. [Google Scholar] [CrossRef] [Scilit]
  51. Mills, R.E.; Luttig, C.T.; Larkins, C.E.; Beauchamp, A.; Tsui, C.; Pittard, W.S.; Devine, S.E. An initial map of insertion and deletion (INDEL) variation in the human genome. Genome Res. 2006, 16, 1182–1190. [Google Scholar] [CrossRef] [Scilit]
  52. Alkan, C.; Kidd, J.M.; Marques-Bonet, T.; Aksay, G.; Antonacci, F.; Hormozdiari, F.; Kitzman, J.O.; Baker, C.; Malig, M.; Mutlu, O.; et al. Personalized copy number and segmental duplication maps using next-generation sequencing. Nat. Genet. 2009, 41, 1061–1067. [Google Scholar] [CrossRef] [Scilit]
  53. Sazanov, A.A.; Romanov, M.N.; Smirnov, A.F. Libraries of large-insert genomic clones as a tool for molecular cytogenetic analysis of avian genome. Russ. J. Genet. 2005, 41, 461–467. [Google Scholar] [CrossRef] [Scilit]
  54. Sazanov, A.A.; Romanov, M.N.; Wardecka, B.; Sazanova, A.L.; Korczak, M.; Stekol’nikova, V.A.; Kozyreva, A.A.; Smirnov, A.F.; Jaszczak, K.; Dodgson, J.B. Chromosomal localization of 15 large insert BAC clones containing three microsatellites on chicken chromosome 4 (GGA4) which refine its centromere position. Anim. Genet. 2005, 36, 161–163. [Google Scholar] [CrossRef] [Scilit]
  55. Matzke, A.; Churakov, G.; Berkes, P.; Arms, E.M.; Kelsey, D.; Brosius, J.; Kriegs, J.O.; Schmitz, J. Retroposon insertion patterns of neoavian birds: Strong evidence for an extensive incomplete lineage sorting era. Mol. Biol. Evol. 2012, 29, 1497–1501. [Google Scholar] [CrossRef] [Scilit]
  56. Rokas, A.; Holland, P.W. Rare genomic changes as a tool for phylogenetics. Trends Ecol. Evol. 2000, 15, 454–459. [Google Scholar] [CrossRef] [Scilit]
  57. Edwards, S.V.; Bryan Jennings, W.; Shedlock, A.M. Phylogenetics of modern birds in the era of genomics. Proc. Biol. Sci. 2005, 272, 979–992. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  58. Griffin, D.K.; Kretschmer, R.; Srikulnath, K.; Singchat, W.; O’Connor, R.E.; Romanov, M.N. Insights into avian molecular cytogenetics—With reptilian comparisons. Mol. Cytogenet. 2024, 17, 24. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  59. Gingrich, J.C.; Boehrer, D.M.; Garnes, J.A.; Johnson, W.; Wong, B.S.; Bergmann, A.; Eveleth, G.G.; Langlois, R.G.; Carrano, A.V. Construction and characterization of human chromosome 2-specific cosmid, fosmid, and PAC clone libraries. Genomics 1996, 32, 65–74. [Google Scholar] [CrossRef] [Scilit]
  60. Azhaguvel, P.; Weng, Y.; Babu, R.; Manickavelu, A.; Saraswathi, D.V.; Balyan, H.S. Fundamentals of physical mapping. In Principles and Practices of Plant Genomics; Kole, C., Abbott, A.G., Eds.; CRC Press: Boca Raton, FL, USA, 2016; Volume 3, pp. 24–62. [Google Scholar] [CrossRef] [Scilit]
  61. Sazanov, A.A.; Romanov, M.N.; Sazanova, A.L.; Tzareva, V.A.; Kozyreva, A.A.; Price, J.A.; Smirnov, A.F.; Dodgson, J.B. Chromosomal Localization of Continuous Genomic Clones in the Chicken with a View of Comparative Mapping. In Genetics in the XXI Century: Current State and Prospects for Development, Proceedings of the III Congress of the Vavilov Society of Geneticists and Selectionists, Moscow, Russia, 6–12 June 2004; Vavilov Society of Geneticists and Selectionists, N.I. Vavilov Institute of General Genetics, M.V., Lomonosov Moscow State University: Moscow, Russia, 2004; Volume 2, p. 271. Available online: https://kar.kent.ac.uk/46505/ (accessed on 17 May 2026).
  62. Janes, D.E.; Valenzuela, N.; Ezaz, T.; Amemiya, C.; Edwards, S.V. Sex chromosome evolution in amniotes: Applications for bacterial artificial chromosome libraries. BioMed Res. Int. 2011, 2011, 132975. [Google Scholar] [CrossRef] [Scilit]
  63. Romanov, M.N.; O’Connor, R.; Skinner, B.M.; Martell, H.; Farré, M.; Larkin, D.M.; Griffin, D.K. Comparative Cytogenomics Enhanced with Bioinformatic Tools Provides Further Insights into Genome Evolution of Birds and Other Amniotes. In Proceedings of the 2nd Annual Food, Nutrition and Agriculture Genomics Congress: Congress Workbook, London, UK, 29–30 April 2015; Abstract 5; Oxford Global Conferences Ltd.: London, UK, 2015; Available online: https://kar.kent.ac.uk/48107/ (accessed on 17 May 2026).
  64. Claeys, J.; Romanov, M.N.; Griffin, D.K. Integrative comparative analysis of avian chromosome evolution by in-silico mapping of the gene ontology of homologous synteny blocks and evolutionary breakpoint regions. Genetica 2023, 151, 167–178. [Google Scholar] [CrossRef] [Scilit]
  65. Romanov, M.N.; Tuttle, E.M.; Houck, M.L.; Modi, W.S.; Chemnick, L.G.; Korody, M.L.; Mork, E.; Otten, C.A.; Renner, T.; Jones, K.C.; et al. The value of avian genomics to the conservation of wildlife. BMC Genom. 2009, 10, S10. [Google Scholar] [CrossRef] [Scilit]
  66. Ryder, O.; Romanov, M.; Stremel, E.; Chemnick, L.; Ballou, J.; Ralls, K.; Mitchell, A.; Thompson, E.; Jones, K. Improving genetic management of California Condors through molecular research. Auk 2007, 124, 36BB. [Google Scholar] [CrossRef] [Scilit]
  67. Ryder, O.A.; Miller, W.; Ralls, K.; Ballou, J.D.; Steiner, C.C.; Mitelberg, A.; Romanov, M.N.; Chemnick, L.G.; Mace, M.; Schuster, S. Whole Genome Sequencing of California Condors Is Now Utilized for Guiding Genetic Management. In International Plant and Animal Genome XXIV Conference, San Diego, CA, USA, 8–13 January 2016; Abstract W741; Scherago International: San Diego, CA, USA, 2016; Available online: http://kar.kent.ac.uk/61072 (accessed on 17 May 2026).
  68. Hogg, C.J.; Ottewell, K.; Latch, P.; Rossetto, M.; Biggs, J.; Gilbert, A.; Richmond, S.; Belov, K. Threatened Species Initiative: Empowering conservation action using genomic resources. Proc. Natl. Acad. Sci. USA 2022, 119, e2115643118. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  69. Capel, S.L.R.; Bouzat, J.L.; Catchen, J.M.; Johnson, J.A.; Dunn, P.O.; Paige, K.N. Evaluating the genome-wide impacts of species translocations: The greater prairie-chicken as a case study. Conserv. Genet. 2022, 23, 179–191. [Google Scholar] [CrossRef] [Scilit]
  70. Guhlin, J.; Le Lec, M.F.; Wold, J.; Koot, E.; Winter, D.; Biggs, P.J.; Galla, S.J.; Urban, L.; Foster, Y.; Cox, M.P.; et al. Species-wide genomics of kākāpō provides tools to accelerate recovery. Nat. Ecol. Evol. 2023, 7, 1693–1705. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  71. Romanov, M.N. California condors Benefit from Genome Studies. CRES Report. 2005. Available online: https://kar.kent.ac.uk/37544/ (accessed on 17 May 2026).
  72. Nam, K.; Mugal, C.; Nabholz, B.; Schielzeth, H.; Wolf, J.B.; Backström, N.; Künstner, A.; Balakrishnan, C.N.; Heger, A.; Ponting, C.P.; et al. Molecular evolution of genes in avian genomes. Genome Biol. 2010, 11, R68. [Google Scholar] [CrossRef] [Scilit]
  73. Backström, N.; Forstmeier, W.; Schielzeth, H.; Mellenius, H.; Nam, K.; Bolund, E.; Webster, M.T.; Öst, T.; Schneider, M.; Kempenaers, B.; et al. The recombination landscape of the zebra finch Taeniopygia guttata genome. Genome Res. 2010, 20, 485. [Google Scholar] [CrossRef] [Scilit]
  74. Smeds, L.; Secomandi, S.; Lee, C.; Chiaromonte, F.; Jarvis, E.D.; Formenti, G.; Makova, K.D. Non-canonical DNA in bird telomere-to-telomere genomes. bioRxiv 2025. [Google Scholar] [CrossRef] [Scilit]
  75. Corval, H.; Ducrest, A.L.; Bachmann Salvy, M.; Burns, A.; Topaloudis, A.; Simon, C.; Cora, E.; Cavaleri, D.; Almasi, B.; Roulin, A.; et al. A chromosome-level, haplotype-resolved genome assembly for the barn owl, Tyto alba. bioRxiv 2026. [Google Scholar] [CrossRef] [Scilit]
  76. Cheng, H.; Jarvis, E.D.; Fedrigo, O.; Koepfli, K.P.; Urban, L.; Gemmell, N.J.; Li, H. Haplotype-resolved assembly of diploid genomes without parental data. Nat. Biotechnol. 2022, 40, 1332–1335. [Google Scholar] [CrossRef] [Scilit]
  77. Sarashetti, P.; Lipovac, J.; Tomas, F.; Šikić, M.; Liu, J. Evaluating data requirements for high-quality haplotype-resolved genomes for creating robust pangenome references. Genome Biol. 2024, 25, 312. [Google Scholar] [CrossRef] [Scilit]
  78. Gross, C.; Potabattula, R.; Cheng, F.; Leuchtenberg, S.; Hartung, H.S.; Kristmann, B.; Buena-Atienza, E.; Casadei, N.; Ossowski, S.; Riess, O. Single-platform nanopore sequencing enables diploid telomere-to-telomere genome assembly and haplotype-resolved 3D chromatin maps. bioRxiv 2026. [Google Scholar] [CrossRef] [Scilit]
  79. Bravo, G.A.; Schmitt, C.J.; Edwards, S.V. What have we learned from the first 500 avian genomes? Annu. Rev. Ecol. Evol. Syst. 2021, 52, 611–639. [Google Scholar] [CrossRef] [Scilit]
  80. Logsdon, G.A.; Vollger, M.R.; Eichler, E.E. Long-read human genome sequencing and its applications. Nat. Rev. Genet. 2020, 21, 597–614. [Google Scholar] [CrossRef] [Scilit]
  81. Bleidorn, C. Third generation sequencing: Technology and its potential impact on evolutionary biodiversity research. Syst. Biodivers. 2016, 14, 1–8. [Google Scholar] [CrossRef] [Scilit]
  82. Schwartz, D.C.; Li, X.; Hernandez, L.I.; Ramnarain, S.P.; Huff, E.J.; Wang, Y.K. Ordered restriction maps of Saccharomyces cerevisiae chromosomes constructed by optical mapping. Science 1993, 262, 110–114. [Google Scholar] [CrossRef] [Scilit]
  83. Cosma, B.M.; Shirali Hossein Zade, R.; Jordan, E.N.; van Lent, P.; Peng, C.; Pillay, S.; Abeel, T. Evaluating long-read de novo assembly tools for eukaryotic genomes: Insights and considerations. GigaScience 2023, 12, giad100. [Google Scholar] [CrossRef] [Scilit]
  84. Okuno, M.; Mizushima, S.; Kuroiwa, A.; Itoh, T. Analysis of sex chromosome evolution in the clade Palaeognathae from phased genome assembly. Genome Biol. Evol. 2021, 13, evab242. [Google Scholar] [CrossRef] [Scilit]
  85. DeRaad, D.A.; Escalona, M.; Benham, P.M.; Marimuthu, M.P.; Sahasrabudhe, R.M.; Nguyen, O.; Chumchim, N.; Beraut, E.; Fairbairn, C.W.; Seligmann, W.; et al. De novo assembly of a chromosome-level reference genome for the California Scrub-Jay, Aphelocoma californica. J. Hered. 2023, 114, 669–680. [Google Scholar] [CrossRef] [Scilit]
  86. Zhou, H.; Huang, X.; Liu, J.; Ding, J.; Xu, K.; Zhu, W.; He, C.; Yang, L.; Zhu, J.; Han, C.; et al. De novo phased genome assembly, annotation and population genotyping of Alectoris chukar. Sci. Data 2024, 11, 162. [Google Scholar] [CrossRef] [Scilit]
  87. Schwartz, D.C. Optical Mapping: New Applications, Advances and Challenges; Thematic Series Published by GigaScience, Collections from GigaScience; Oxford University Press: Oxford, UK, 2014; Available online: https://academic.oup.com/gigascience/pages/optical_mapping_new_applications_advances_challenges (accessed on 17 May 2026).
  88. Sutton, J.T.; Helmkampf, M.; Steiner, C.C.; Bellinger, M.R.; Korlach, J.; Hall, R.; Baybayan, P.; Muehling, J.; Gu, J.; Kingan, S.; et al. A high-quality, long-read de novo genome assembly to aid conservation of Hawaii’s last remaining crow species. Genes 2018, 9, 393. [Google Scholar] [CrossRef] [Scilit]
  89. Peona, V.; Weissensteiner, M.H.; Suh, A. How complete are “complete” genome assemblies?—An avian perspective. Mol. Ecol. Resour. 2018, 18, 1188–1195. [Google Scholar] [CrossRef] [Scilit]
  90. Huttener, R.; Thorrez, L.; Veld, T.I.; Granvik, M.; Van Lommel, L.; Waelkens, E.; Derua, R.; Lemaire, K.; Goyvaerts, L.; De Coster, S.; et al. Sequencing refractory regions in bird genomes are hotspots for accelerated protein evolution. BMC Ecol. Evol. 2021, 21, 176. [Google Scholar] [CrossRef] [Scilit]
  91. Korlach, J.; Gedman, G.; Kingan, S.B.; Chin, C.-S.; Howard, J.T.; Audet, J.-N.; Cantin, L.; Jarvis, E.D. De novo PacBio long-read and phased avian genome assemblies correct and add to reference genes generated with intermediate and short reads. GigaScience 2017, 6, gix085. [Google Scholar] [CrossRef] [Scilit]
  92. He, K.; Minias, P.; Dunn, P.O. Long-read genome assemblies reveal extraordinary variation in the number and structure of MHC loci in birds. Genome Biol. Evol. 2021, 13, evaa270. [Google Scholar] [CrossRef] [Scilit]
  93. Wang, J.; Xi, Y.; Ma, S.; Qi, J.; Li, J.; Zhang, R.; Han, C.; Li, L.; Wang, J.; Liu, H. Single-molecule long-read sequencing reveals the potential impact of posttranscriptional regulation on gene dosage effects on the avian Z chromosome. BMC Genom. 2022, 23, 122. [Google Scholar] [CrossRef] [Scilit]
  94. Howe, K.; Wood, J.M. Using optical mapping data for the improvement of vertebrate genome assemblies. GigaScience 2015, 4, s13742-015-0052-y. [Google Scholar] [CrossRef] [Scilit]
  95. Zhang, J.; Li, C.; Zhou, Q.; Zhang, G. Improving the ostrich genome assembly using optical mapping data. GigaScience 2015, 4, s13742-015-0062–0069. [Google Scholar] [CrossRef] [Scilit]
  96. Huo, W.; Ling, W.; Wang, Z.; Li, Y.; Zhou, M.; Ren, M.; Li, X.; Li, J.; Xia, Z.; Liu, X.; et al. Miniaturized DNA sequencers for personal use: Unreachable dreams or achievable goals. Front. Nanotechnol. 2021, 3, 628861. [Google Scholar] [CrossRef] [Scilit]
  97. Rhoads, A.; Au, K.F. PacBio sequencing and its applications. Genom. Proteom. Bioinform. 2015, 13, 278–289. [Google Scholar] [CrossRef] [Scilit]
  98. Weissensteiner, M.H.; Bunikis, I.; Catalán, A.; Francoijs, K.-J.; Knief, U.; Heim, W.; Peona, V.; Pophaly, S.D.; Sedlazeck, F.J.; Suh, A.; et al. Discovery and population genomics of structural variation in a songbird genus. Nat. Commun. 2020, 11, 3403. [Google Scholar] [CrossRef] [Scilit]
  99. Lundberg, M.; Mackintosh, A.; Petri, A.; Bensch, S. Inversions maintain differences between migratory phenotypes of a songbird. Nat. Commun. 2023, 14, 452. [Google Scholar] [CrossRef] [Scilit]
  100. Zhang, Z.; Ni, Z.; Li, T.; Ning, M.; Gao, C.; Hu, J.; Han, M.; Yang, J.; Wu, F.; Chen, L.; et al. Nine high-quality Anas genomes provide insights into Anas evolution and domestication. Cell Rep. 2025, 44, 115477. [Google Scholar] [CrossRef] [Scilit]
  101. Damas, J.; Kim, J.; Farré, M.; Griffin, D.K.; Larkin, D.M. Reconstruction of avian ancestral karyotypes reveals differences in the evolutionary history of macro-and microchromosomes. Genome Biol. 2018, 19, 155. [Google Scholar] [CrossRef] [Scilit]
  102. Ezaz, T.; Stiglec, R.; Veyrunes, F.; Graves, J.A.M. Relationships between vertebrate ZW and XY sex chromosome systems. Curr. Biol. 2006, 16, R736–R743. [Google Scholar] [CrossRef] [Scilit]
  103. Irwin, D.E. Sex chromosomes and speciation in birds and other ZW systems. Mol. Ecol. 2018, 27, 3831–3851. [Google Scholar] [CrossRef] [Scilit]
  104. Xu, L.; Zhou, Q. The female-specific W chromosomes of birds have conserved gene contents but are not feminized. Genes 2020, 11, 1126. [Google Scholar] [CrossRef] [Scilit]
  105. Schartl, M.; Schmid, M.; Nanda, I. Dynamics of vertebrate sex chromosome evolution: From equal size to giants and dwarfs. Chromosoma 2016, 125, 553–571. [Google Scholar] [CrossRef] [Scilit]
  106. Ellegren, H. The evolutionary genomics of birds. Annu. Rev. Ecol. Evol. Syst. 2013, 44, 239–259. [Google Scholar] [CrossRef] [Scilit]
  107. Deakin, J.E.; Ezaz, T. Tracing the evolution of amniote chromosomes. Chromosoma 2014, 123, 201–216. [Google Scholar] [CrossRef] [Scilit]
  108. Bellott, D.W.; Skaletsky, H.; Pyntikova, T.; Mardis, E.R.; Graves, T.; Kremitzki, C.; Brown, L.G.; Rozen, S.; Warren, W.C.; Wilson, R.K.; et al. Convergent evolution of chicken Z and human X chromosomes by expansion and gene acquisition. Nature 2010, 466, 612–616. [Google Scholar] [CrossRef] [Scilit]
  109. Blagoveshchenskiĭ, I.I.; Sazanova, A.L.; Stekol’nikova, V.A.; Fomichev, K.A.; Barkova, O.I.; Romanov, M.N.; Sazanov, A.A. Investigation of pseudoautosomal and bordering regions in avian Z and W chromosomes with the use of large insert genomic BAC clones. Genetika 2011, 47, 312–319. [Google Scholar]
  110. Tomaszkiewicz, M.; Medvedev, P.; Makova, K.D. Y and W chromosome assemblies: Approaches and discoveries. Trends Genet. 2017, 33, 266–282. [Google Scholar] [CrossRef] [Scilit]
  111. Torgasheva, A.A.; Malinovskaya, L.P.; Zadesenets, K.S.; Karamysheva, T.V.; Kizilova, E.A.; Akberdina, E.A.; Pristyazhnyuk, I.E.; Shnaider, E.P.; Volodkina, V.A.; Saifitdinova, A.F.; et al. Germline-restricted chromosome (GRC) is widespread among songbirds. Proc. Natl. Acad. Sci. USA 2019, 116, 11845–11850. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  112. Sotelo-Muñoz, M.; Poignet, M.; Albrecht, T.; Kauzál, O.; Dedukh, D.; Schlebusch, S.A.; Janko, K.; Reifová, R. Germline-restricted chromosome shows remarkable variation in size among closely related passerine species. Chromosoma 2022, 131, 77–86. [Google Scholar] [CrossRef] [Scilit]
  113. Kinsella, C.M.; Ruiz-Ruano, F.J.; Dion-Côté, A.M.; Charles, A.J.; Gossmann, T.I.; Cabrero, J.; Kappei, D.; Hemmings, N.; Simons, M.J.; Camacho, J.P.M. Programmed DNA elimination of germline development genes in songbirds. Nat. Commun. 2019, 10, 5468. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  114. Schlebusch, S.A.; Rídl, J.; Poignet, M.; Ruiz-Ruano, F.J.; Reif, J.; Pajer, P.; Pačes, J.; Albrecht, T.; Suh, A.; Reifová, R. Rapid gene content turnover on the germline-restricted chromosome in songbirds. Nat. Commun. 2023, 14, 4579. [Google Scholar] [CrossRef] [Scilit]
  115. Waters, P.D.; Patel, H.R.; Ruiz-Herrera, A.; Álvarez-González, L.; Lister, N.C.; Simakov, O.; Ezaz, T.; Kaur, P.; Frere, C.; Grützner, F.; et al. Microchromosomes are building blocks of bird, reptile, and mammal chromosomes. Proc. Natl. Acad. Sci. USA 2021, 118, e2112494118. [Google Scholar] [CrossRef] [Scilit]
  116. Zhou, Q.; Zhang, J.; Bachtrog, D.; An, N.; Huang, Q.; Jarvis, E.D.; Gilbert, M.T.P.; Zhang, G. Complex evolutionary trajectories of sex chromosomes across bird taxa. Science 2014, 346, 1246338. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  117. Peona, V.; Palacios-Gimenez, O.M.; Blommaert, J.; Liu, J.; Haryoko, T.; Jønsson, K.A.; Irestedt, M.; Zhou, Q.; Jern, P.; Suh, A. The avian W chromosome is a refugium for endogenous retroviruses with likely effects on female-biased mutational load and genetic incompatibilities. Philos. Trans. R. Soc. B Biol. Sci. 2021, 376, 20200186. [Google Scholar] [CrossRef] [Scilit]
  118. Borodin, P.; Chen, A.; Forstmeier, W.; Fouché, S.; Malinovskaya, L.; Pei, Y.; Reifová, R.; Ruiz-Ruano, F.J.; Schlebusch, S.A.; Sotelo-Muñoz, M.; et al. Mendelian nightmares: The germline-restricted chromosome of songbirds. Chromosome Res. 2022, 30, 255–272. [Google Scholar] [CrossRef] [Scilit]
  119. Lagunov, T.; Gridina, M.; Nurislamov, A.; Kulikova, T.; Maslova, A.; Konstantinov, V.; Popov, A.; Krasikova, A.; Fishman, V. The 3D genomics of lampbrush chromosomes highlights the role of active transcription in chromatin organization. Nucleic Acids Res. 2026, 54, gkag316. [Google Scholar] [CrossRef] [Scilit]
  120. Galkina, S.; Deryusheva, S.; Fillon, V.; Vignal, A.; Crooijmans, R.; Groenen, M.; Rodionov, A.; Gaginskaya, E. FISH on avian lampbrush chromosomes produces higher resolution gene mapping. Genetica 2006, 128, 241–251. [Google Scholar] [CrossRef] [Scilit]
  121. Krasikova, A.; Deryusheva, S.; Galkina, S.; Kurganova, A.; Evteev, A.; Gaginskaya, E. On the positions of centromeres in chicken lampbrush chromosomes. Chromosome Res. 2006, 14, 777–789. [Google Scholar] [CrossRef] [Scilit]
  122. Romanov, M.N.; Sazanov, A.A.; Moiseyeva, I.G.; Smirnov, A.F. Poultry. In Genome Mapping and Genomics in Animals, Volume 3: Genome Mapping and Genomics in Domestic Animals; Cockett, N.E., Kole, C., Eds.; Springer: Berlin/Heidelberg, Germany, 2009; pp. 75–141. [Google Scholar] [CrossRef] [Scilit]
  123. Dodgson, J.B.; Romanov, M.N. The Chicken Genome: From Maps to Sequence. In Proceedings of the 8th International Symposium on Avian Endocrinology: Symposium Talk and Plenary Lecture Abstracts, Scottsdale, AZ, USA, 6–11 June 2004; Abstract T26; Arizona State University: Scottsdale, AZ, USA, 2004; Available online: https://kar.kent.ac.uk/46516/ (accessed on 17 May 2026).
  124. Sazanov, A.A.; Sazanova, A.L.; Romanov, M.N.; Stekol’nikova, V.A.; Malewski, T.; Korczak, M.; Jaszczak, K.; Smirnov, A.F. Molecular Organization of Chicken Genome. In Proceedings of the Genomic and Microarray Analysis in Biology and Medicine, Sucha Beskidzka, Poland, 25–28 June 2005; p. 26. Available online: https://kar.kent.ac.uk/46616/ (accessed on 17 May 2026).
  125. Romanov, M.N.; Sazanov, A.A.; Smirnov, A.F. First century of chicken gene study and mapping—A look back and forward. Worlds Poult. Sci. J. 2004, 60, 19–41. [Google Scholar] [CrossRef] [Scilit]
  126. Carbone, L.; Nergadze, S.G.; Magnani, E.; Misceo, D.; Francesca Cardone, M.; Roberto, R.; Bertoni, L.; Attolini, C.; Francesca Piras, M.; de Jong, P.; et al. Evolutionary movement of centromeres in horse, donkey, and zebra. Genomics 2006, 87, 777–782. [Google Scholar] [CrossRef] [Scilit]
  127. Chowdhary, B.P.; Raudsepp, T.; Frönicke, L.; Scherthan, H. Emerging patterns of comparative genome organization in some mammalian species as revealed by Zoo-FISH. Genome Res. 1998, 8, 577–589. [Google Scholar] [CrossRef] [Scilit]
  128. Ray-Chaudhuri, R. Cytotaxonomy and chromosome evolution in birds. In Cytotaxonomy and Vertebrate Evolution; Chiarelli, A.B., Capanna, E., Eds.; Academic Press: New York, NY, USA, 1973; pp. 425–483. [Google Scholar]
  129. Takagi, N.; Sasaki, M. A phylogenetic study of bird karyotypes. Chromosoma 1974, 46, 91–120. [Google Scholar] [CrossRef] [Scilit]
  130. Tegelström, H.; Ryttman, H. Chromosomes in birds (Aves): Evolutionary implications of macro-and microchromosome numbers and lengths. Hereditas 1981, 94, 225–233. [Google Scholar] [CrossRef] [Scilit]
  131. Tegelström, H.; Ebenhard, T.; Ryttman, H. Rate of karyotype evolution and speciation in birds. Hereditas 1983, 98, 235–239. [Google Scholar] [CrossRef] [Scilit]
  132. Kretschmer, R.; Ferguson-Smith, M.; de Oliveira, E. Karyotype evolution in birds: From conventional staining to chromosome painting. Genes 2018, 9, 181. [Google Scholar] [CrossRef] [Scilit]
  133. Kretschmer, R.; Gunski, R.J.; Garnero, A.d.V.; Furo, I.d.O.; O’Brien, P.C.M.; Ferguson-Smith, M.A.; de Oliveira, E.H.C. Molecular cytogenetic characterization of multiple intrachromosomal rearrangements in two representatives of the genus Turdus (Turdidae, Passeriformes). PLoS ONE 2014, 9, e103338. [Google Scholar] [CrossRef] [Scilit]
  134. Skinner, B.M.; Griffin, D.K. Intrachromosomal rearrangements in avian genome evolution: Evidence for regions prone to breakpoints. Heredity 2012, 108, 37–41. [Google Scholar] [CrossRef] [Scilit]
  135. Robertson, W.R.B. Chromosome studies. I. Taxonomic relationships shown in the chromosomes of Tettigidae and Acrididae. V-shaped chromosomes and their significance in Acrididae, Locustidae and Gryllidae: Chromosome and variation. J. Morphol. 1916, 27, 179–331. [Google Scholar] [CrossRef] [Scilit]
  136. Schmid, M.; Nanda, I.; Guttenbach, M.; Steinlein, C.; Hoehn, M.; Schartl, M.; Haaf, T.; Weigend, S.; Fries, R.; Buerstedde, J.-M.; et al. First Report on Chicken Genes and Chromosomes 2000. Cytogenet. Genome Res. 2000, 90, 169–218. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  137. Schmid, M.; Nanda, I.; Burt, D.W. Second Report on Chicken Genes and Chromosomes 2005. Cytogenet. Genome Res. 2005, 109, 415–479. [Google Scholar] [CrossRef] [Scilit]
  138. Raudsepp, T.; Houck, M.L.; O’Brien, P.C.; Ferguson-Smith, M.A.; Ryder, O.A.; Chowdhary, B.P. Cytogenetic analysis of California condor (Gymnogyps californianus) chromosomes: Comparison with chicken (Gallus gallus) macrochromosomes. Cytogenet. Genome Res. 2002, 98, 54–60. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  139. Itoh, Y.; Arnold, A.P. Chromosomal polymorphism and comparative painting analysis in the zebra finch. Chromosome Res. 2005, 13, 47–56. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  140. Shibusawa, M.; Nishida-Umehara, C.; Masabanda, J.; Griffin, D.K.; Isobe, T.; Matsuda, Y. Chromosome Rearrangements between chicken and guinea fowl defined by comparative chromosome painting and FISH mapping of DNA clones. Cytogenet. Genome Res. 2002, 98, 225–230. [Google Scholar] [CrossRef] [Scilit]
  141. Sazanov, A.A.; Sazanova, A.L.; Stekolnikova, V.A.; Kozyreva, A.A.; Smirnov, A.F.; Romanov, M.N.; Dodgson, J.B. Chromosomal localization of CTSL: Expanding of the region of evolutionary conservation between GGAZ and HSA9. Anim. Genet. 2004, 35, 260. [Google Scholar] [CrossRef] [Scilit]
  142. Sazanov, A.A.; Sazanova, A.L.; Tzareva, V.A.; Kozyreva, A.A.; Smirnov, A.F.; Romanov, M.N.; Price, J.A.; Dodgson, J.B. Chromosomal localization of three GGA4 genes using BAC-based FISH mapping: A region of conserved synteny between the chicken and human genomes. Hereditas 2004, 140, 249–251. [Google Scholar] [CrossRef] [Scilit]
  143. Derjusheva, S.; Kurganova, A.; Habermann, F.; Gaginskaya, E. High chromosome conservation detected by comparative chromosome painting in chicken, pigeon and passerine birds. Chromosome Res. 2004, 12, 715–723. [Google Scholar] [CrossRef] [Scilit]
  144. Kasai, F.; Garcia, C.; Arruga, M.V.; Ferguson-Smith, M.A. Chromosome homology between chicken (Gallus gallus domesticus) and the red-legged partridge (Alectoris rufa); evidence of the occurrence of a neocentromere during evolution. Cytogenet. Genome Res. 2003, 102, 326–330. [Google Scholar] [CrossRef] [Scilit]
  145. Fillon, V.; Vignoles, M.; Crooijmans, R.P.M.A.; Groenen, M.A.M.; Zoorob, R.; Vignal, A. FISH mapping of 57 BAC clones reveals strong conservation of synteny between Galliformes and Anseriformes. Anim. Genet. 2007, 38, 303–307. [Google Scholar] [CrossRef] [Scilit]
  146. Zhang, Y.; Zhang, X.; O’Hare, T.H.; Payne, W.S.; Dong, J.J.; Scheuring, C.F.; Zhang, M.; Huang, J.J.; Lee, M.K.; Delany, M.E.; et al. A comparative physical map reveals the pattern of chromosomal evolution between the turkey (Meleagris gallopavo) and chicken (Gallus gallus) genomes. BMC Genom. 2011, 12, 447. [Google Scholar] [CrossRef] [Scilit]
  147. Aggrey, S.E.; Zhou, H.; Tixier-Boichard, M.; Rhoads, D.D. (Eds.) Advances in Poultry Genetics and Genomics; Burleigh Dodds Science Publishing Limited: Cambridge, UK, 2020. [Google Scholar]
  148. Seligmann, I.C.A.; Furo, I.d.O.; dos Santos, M.d.S.; Gunski, R.J.; Garnero, A.d.V.; Silva, F.A.O.; O’Brien, P.; Ferguson-Smith, M.; Kretschmer, R.; de Oliveira, E.H.C. Comparative chromosome painting in three Pelecaniformes species (Aves): Exploring the role of macro and microchromosome fusions in karyotypic evolution. PLoS ONE 2023, 18, e0294776. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  149. Nishida, C.; Ishijima, J.; Kosaka, A.; Tanabe, H.; Habermann, F.A.; Griffin, D.K.; Matsuda, Y. Characterization of chromosome structures of Falconinae (Falconidae, Falconiformes, Aves) by chromosome painting and delineation of chromosome rearrangements during their differentiation. Chromosome Res. 2008, 16, 171–181. [Google Scholar] [CrossRef] [Scilit]
  150. Furo, I.d.O.; Kretschmer, R.; O’Brien, P.C.; Pereira, J.C.; Garnero, A.d.V.; Gunski, R.J.; O’Connor, R.E.; Griffin, D.K.; Gomes, A.J.B.; Ferguson-Smith, M.A.; et al. Chromosomal evolution in the phylogenetic context: A remarkable karyotype reorganization in neotropical parrot Myiopsitta monachus (Psittacidae). Front. Genet. 2020, 11, 721. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  151. Joseph, S.; O’Connor, R.; Al Mutery, A.; Watson, M.; Larkin, D.; Griffin, D. Chromosome level genome assembly and comparative genomics between three falcon species reveals an unusual pattern of genome organisation. Diversity 2018, 10, 113. [Google Scholar] [CrossRef] [Scilit]
  152. Nanda, I.; Karl, E.; Volobouev, V.; Griffin, D.K.; Schartl, M.; Schmid, M. Extensive gross genomic rearrangements between chicken and Old World vultures (Falconiformes: Accipitridae). Cytogenet. Genome Res. 2006, 112, 286–295. [Google Scholar] [CrossRef] [Scilit]
  153. De Oliveira, E.H.C.; Habermann, F.A.; Lacerda, O.; Sbalqueiro, I.J.; Wienberg, J.; Müller, S. Chromosome reshuffling in birds of prey: The karyotype of the world’s largest eagle (Harpy eagle, Harpia harpyja) compared to that of the chicken (Gallus gallus). Chromosoma 2005, 114, 338–343. [Google Scholar] [CrossRef] [Scilit]
  154. Modi, W.S.; Romanov, M.; Green, E.D.; Ryder, O. Molecular cytogenetics of the California condor: Evolutionary and conservation implications. Cytogenet. Genome Res. 2009, 127, 26–32. [Google Scholar] [CrossRef] [Scilit]
  155. Sazanov, A.A.; Sazanova, A.L.; Nefedov, M.D.; Griffin, D.K.; Romanov, M.N. A pair of gametologous genes provides further insights into avian comparative cytogenomics. Biologia 2023, 78, 2737–2746. [Google Scholar] [CrossRef] [Scilit]
  156. Dalloul, R.A.; Long, J.A.; Zimin, A.V.; Aslam, L.; Beal, K.; Ann Blomberg, L.; Bouffard, P.; Burt, D.W.; Crasta, O.; Crooijmans, R.P.M.A.; et al. Multi-platform next-generation sequencing of the domestic turkey (Meleagris gallopavo): Genome assembly and analysis. PLoS Biol. 2010, 8, e1000475. [Google Scholar] [CrossRef] [Scilit]
  157. Warren, W.C.; Clayton, D.F.; Ellegren, H.; Arnold, A.P.; Hillier, L.W.; Künstner, A.; Searle, S.; White, S.; Vilella, A.J.; Fairley, S.; et al. The Genome of a songbird. Nature 2010, 464, 757–762. [Google Scholar] [CrossRef] [Scilit]
  158. Völker, M.; Backström, N.; Skinner, B.M.; Langley, E.J.; Bunzey, S.K.; Ellegren, H.; Griffin, D.K. Copy number variation, chromosome rearrangement, and their association with recombination during avian evolution. Genome Res. 2010, 20, 503–511. [Google Scholar] [CrossRef] [Scilit]
  159. Choudhuri, J.V.; Schleiermacher, C.; Kurtz, S.; Giegerich, R. GenAlyzer: Interactive visualization of sequence similarities between entire genomes. Bioinformatics 2004, 20, 1964–1965. [Google Scholar] [CrossRef] [Scilit]
  160. Romanov, M.N.; Dodgson, J.B. Development of a Physical and Comparative Map of the Turkey Genome. In Proceedings of the International Plant and Animal Genome XIII Conference, San Diego, CA, USA, 15–19 January 2005; Abstract W297; Scherago International: San Diego, CA, USA, 2005; p. 69. Available online: https://kar.kent.ac.uk/46542/ (accessed on 17 May 2026).
  161. Ezaz, T.; Moritz, B.; Waters, P.; Marshall Graves, J.A.; Georges, A.; Sarre, S.D. The ZW sex microchromosomes of an Australian dragon lizard share no homology with those of other reptiles or birds. Chromosome Res. 2009, 17, 965–973. [Google Scholar] [CrossRef] [Scilit]
  162. Prum, R.O.; Berv, J.S.; Dornburg, A.; Field, D.J.; Townsend, J.P.; Lemmon, E.M.; Lemmon, A.R. A comprehensive phylogeny of birds (Aves) using targeted next-generation DNA sequencing. Nature 2015, 526, 569–573. [Google Scholar] [CrossRef] [Scilit]
  163. Scherf, B.D. (Ed.) World Watch List for Domestic Animal Diversity, 3rd ed.; Food and Agriculture Organization of the United Nations: Rome, Italy, 2000; Available online: https://www.fao.org/4/x8750e/x8750e00.htm (accessed on 17 May 2026).
  164. Nishida-Umehara, C.; Tsuda, Y.; Ishijima, J.; Ando, J.; Fujiwara, A.; Matsuda, Y.; Griffin, D.K. The molecular basis of chromosome orthologies and sex chromosomal differentiation in palaeognathous birds. Chromosome Res. 2007, 15, 721–734. [Google Scholar] [CrossRef] [Scilit]
  165. Liu, J.; Wang, Z.; Li, J.; Xu, L.; Liu, J.; Feng, S.; Guo, C.; Chen, S.; Ren, Z.; Rao, J.; et al. A new emu genome illuminates the evolution of genome configuration and nuclear architecture of avian chromosomes. Genome Res. 2021, 31, 497–511. [Google Scholar] [CrossRef] [Scilit]
  166. Sackton, T.B.; Grayson, P.; Cloutier, A.; Hu, Z.; Liu, J.S.; Wheeler, N.E.; Gardner, P.P.; Clarke, J.A.; Baker, A.J.; Clamp, M.; et al. Convergent regulatory evolution and loss of flight in paleognathous birds. Science 2019, 364, 74–78. [Google Scholar] [CrossRef] [Scilit]
  167. Corbo, M.; Damas, J.; Bursell, M.G.; Lewin, H.A. Conservation of chromatin conformation in carnivores. Proc. Natl. Acad. Sci. USA 2022, 119, e2120555119. [Google Scholar] [CrossRef] [Scilit]
  168. Hoencamp, C.; Dudchenko, O.; Elbatsh, A.M.; Brahmachari, S.; Raaijmakers, J.A.; van Schaik, T.; Sedeño Cacciatore, Á.; Contessoto, V.G.; van Heesbeen, R.G.; van den Broek, B.; et al. 3D genomics across the tree of life reveals condensin II as a determinant of architecture type. Science 2021, 372, 984–989. [Google Scholar] [CrossRef] [Scilit]
  169. Álvarez-González, L.; Burden, F.; Doddamani, D.; Malinverni, R.; Leach, E.; Marín-García, C.; Marín-Gual, L.; Gubern, A.; Vara, C.; Paytuví-Gallart, A.; et al. 3D chromatin remodelling in the germ line modulates genome evolutionary plasticity. Nat. Commun. 2022, 13, 2608. [Google Scholar] [CrossRef] [Scilit]
  170. Edwards, S.V.; Cloutier, A.; Cockburn, G.; Driver, R.; Grayson, P.; Katoh, K.; Baldwin, M.W.; Sackton, T.B.; Baker, A.J. A nuclear genome assembly of an extinct flightless bird, the little bush moa. Sci. Adv. 2024, 10, eadj6823. [Google Scholar] [CrossRef] [Scilit]
  171. Romanov, M.N.; Da, Y.; Chemnick, L.G.; Thomas, S.M.; Dandekar, S.S.; Papp, J.C.; Ryder, O.A. Towards a genetic linkage map of the California condor, an endangered New World vulture species. Animals 2022, 12, 3266. [Google Scholar] [CrossRef] [Scilit]
  172. Banks, R.C.; Fitzpatrick, J.W.; Howell, T.R.; Johnson, N.K.; Monroe, B.L.; Ouellet, H.; Remsen, J.V.; Storer, R.W. Forty-first supplement to the American Ornithologists’ Union Check-List of North American Birds. Auk 1997, 114, 542–552. [Google Scholar] [CrossRef] [Scilit]
  173. Ericson, P.G.P.; Anderson, C.L.; Britton, T.; Elzanowski, A.; Johansson, U.S.; Källersjö, M.; Ohlson, J.I.; Parsons, T.J.; Zuccon, D.; Mayr, G. Diversification of Neoaves: Integration of molecular sequence data and fossils. Biol. Lett. 2006, 2, 543–547. [Google Scholar] [CrossRef] [Scilit]
  174. Chesser, R.T.; Burns, K.J.; Cicero, C.; Dunn, J.L.; Kratter, A.W.; Lovette, I.J.; Rasmussen, P.C.; Remsen, J.V.; Rising, J.D.; Stotz, D.F.; et al. Fifty-seventh supplement to the American Ornithologists’ Union Check-List of North American Birds. Auk 2016, 133, 544–560. [Google Scholar] [CrossRef] [Scilit]
  175. Snyder, N.F.; Snyder, H. Introduction to the California Condor; Volume 81 of California Natural History; University of California Press: Berkeley, CA, USA, 2005. [Google Scholar] [CrossRef] [Scilit]
  176. Gleghorn, L.; Ramesar, R.; Beighton, P.; Wallis, G. A mutation in the variable repeat region of the aggrecan gene (AGC1) causes a form of spondyloepiphyseal dysplasia associated with severe, premature osteoarthritis. Am. J. Hum. Genet. 2005, 77, 484–490. [Google Scholar] [CrossRef] [Scilit]
  177. Li, H.; Schwartz, N.B.; Vertel, B.M. cDNA cloning of chick cartilage chondroitin sulfate (aggrecan) core protein and identification of a stop codon in the aggrecan gene associated with the chondrodystrophy, nanomelia. J. Biol. Chem. 1993, 268, 23504–23511. [Google Scholar] [CrossRef] [Scilit]
  178. Keyser, C.; Pfitzinger, H.; Montagnon, D.; Schlee, M.; Ludes, B.; Mangin, P. First isolation of tandemly repeated DNA sequences in New World vultures and phylogenetic implications. Genome 1996, 39, 31–39. [Google Scholar] [CrossRef] [Scilit]
  179. Ryder, O.A.; Thomas, S.; Judson, J.M.; Romanov, M.N.; Dandekar, S.; Papp, J.C.; Sidak-Loftis, L.C.; Walker, K.; Stalis, I.H.; Mace, M.; et al. Facultative parthenogenesis in California condors. J. Hered. 2021, 112, 569–574. [Google Scholar] [CrossRef] [Scilit]
  180. Robinson, J.A.; Bowie, R.C.K.; Dudchenko, O.; Aiden, E.L.; Hendrickson, S.L.; Steiner, C.C.; Ryder, O.A.; Mindell, D.P.; Wall, J.D. Genome-wide diversity in the California condor tracks its prehistoric abundance and decline. Curr. Biol. 2021, 31, 2939–2946.e5. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  181. Ryder, O.; Chemnick, L.G.; Thomas, S.; Martin, J.; Romanov, M.; Ralls, K.; Ballou, J.D.; Mace, M.; Ratan, A.; Miller, W.; et al. Supporting California Condor Conservation Management through Analysis of Species-wide Whole Genome Sequence Variation. In International Plant and Animal Genome XXII Conference, San Diego, CA, USA, 11–15 January 2014; Abstract W635; Scherago International: San Diego, CA, USA, 2014; Available online: https://kar.kent.ac.uk/46698 (accessed on 17 May 2026).
  182. Trail, P.W. Identifying Bald versus Golden Eagle bones: A primer for wildlife biologists and law enforcement officers. J. Fish Wildl. Manag. 2017, 8, 596–610. [Google Scholar] [CrossRef] [Scilit]
  183. Mindell, D.P.; Fuchs, J.; Johnson, J.A. Phylogeny, taxonomy, and geographic diversity of diurnal raptors: Falconiformes, Accipitriformes, and Cathartiformes. In Birds of Prey; Sarasola, J.H., Grande, J.M., Negro, J.J., Eds.; Springer: Cham, Switzerland, 2018; pp. 3–32. [Google Scholar] [CrossRef] [Scilit]
  184. McClure, C.J.; Dunn, L.; Buechley, E.R.; Juergens, P.; Oleyar, D.; Goodrich, L.J.; Therrien, J.F. Conservation assessment of raptors within the USA and Canada. Biol. Conserv. 2022, 272, 109633. [Google Scholar] [CrossRef] [Scilit]
  185. De Boer, L.E.M.; Sinoo, R.P. A karyological study of Accipitridae (Aves: Falconiformes), with karyotypic descriptions of 16 species new to cytology. Genetica 1984, 65, 89–107. [Google Scholar] [CrossRef] [Scilit]
  186. Jarvis, E.D.; Mirarab, S.; Aberer, A.J.; Li, B.; Houde, P.; Li, C.; Ho, S.Y.W.; Faircloth, B.C.; Nabholz, B.; Howard, J.T.; et al. Phylogenomic analyses data of the Avian Phylogenomics Project. GigaScience 2015, 4, s13742-014-0038-1. [Google Scholar] [CrossRef] [Scilit]
  187. Warren, W.; Jarvis, E.D.; Wilson, R.K.; Howard, J.T.; Gilbert, M.P.; Zhang, G.; The Avian Genome Consortium. Genomic data of the Bald Eagle (Haliaeetus leucocephalus). Gigasci. Database 2014. [Google Scholar] [CrossRef] [Scilit]
  188. Judkins, M.E.; Couger, B.M.; Warren, W.C.; Van Den Bussche, R.A. A 50K SNP array reveals genetic structure for bald eagles (Haliaeetus leucocephalus). Conserv. Genet. 2020, 21, 65–76. [Google Scholar] [CrossRef] [Scilit]
  189. Johansson, U.S.; Irestedt, M.; Qu, Y.; Ericson, P.G.P. Phylogenetic relationships of rollers (Coraciidae) based on complete mitochondrial genomes and fifteen nuclear genes. Mol. Phylogenet. Evol. 2018, 126, 17–22. [Google Scholar] [CrossRef] [Scilit]
  190. Belterman, R.H.R.; De Boer, L.E.M. A karyological study of 55 species of birds, including karyotypes of 39 species new to cytology. Genetica 1984, 65, 39–82. [Google Scholar] [CrossRef] [Scilit]
  191. National Center for Biotechnology Information (NCBI). BioProject. Coracias benghalensis (Indian roller); Accession: PRJNA921248. ID: 921248; National Library of Medicine: Bethesda, MD, USA, 2023. Available online: https://www.ncbi.nlm.nih.gov/bioproject/?term=PRJNA921248 (accessed on 17 May 2026).
  192. Romanov, M.N. Microchromosome Organization in Birds. Encyclopedia (Online). Entry 30520. 2022. Available online: https://encyclopedia.pub/entry/30520 (accessed on 17 May 2026).
  193. Huang, Z.; Furo, I.d.O.; Liu, J.; Peona, V.; Gomes, A.J.B.; Cen, W.; Huang, H.; Zhang, Y.; Chen, D.; Xue, T.; et al. Recurrent chromosome reshuffling and the evolution of neo-sex chromosomes in parrots. Nat. Commun. 2022, 13, 944. [Google Scholar] [CrossRef] [Scilit]
  194. Wang, J.; Su, W.; Hu, Y.; Li, S.; O’Brien, P.C.M.; Ferguson-Smith, M.A.; Yang, F.; Nie, W. Comparative chromosome maps between the stone curlew and three ciconiiform species (the grey heron, little egret and crested ibis). BMC Ecol. Evol. 2022, 22, 23. [Google Scholar] [CrossRef] [Scilit]
  195. Xu, L.; Ren, Y.; Wu, J.; Cui, T.; Dong, R.; Huang, C.; Feng, Z.; Zhang, T.; Yang, P.; Yuan, J.; et al. Evolution and expression patterns of the neo-sex chromosomes of the crested ibis. Nat. Commun. 2024, 15, 1670. [Google Scholar] [CrossRef] [Scilit]
  196. Belterman, R.H.R.; De Boer, L.E.M. A miscellaneous collection of bird karyotypes. Genetica 1990, 83, 17–29. [Google Scholar] [CrossRef] [Scilit]
  197. De Boer, L.E.M.; Van Brink, J.M. Cytotaxonomy of the Ciconiiformes (Aves), with karyotypes of eight species new to cytology. Cytogenet. Genome Res. 1982, 34, 19–34. [Google Scholar] [CrossRef] [Scilit]
  198. Kretschmer, R.; Franz, I.; de Souza, M.S.; Garnero, A.d.V.; Gunski, R.J.; de Oliveira, E.H.C.; O’Connor, R.E.; Griffin, D.K.; de Freitas, T.R.O. Cytogenetic evidence clarifies the phylogeny of the family Rhynchocyclidae (Aves: Passeriformes). Cells 2021, 10, 2650. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  199. Kretschmer, R.; de Souza, M.S.; Gunski, R.J.; Garnero, A.d.V.; de Freitas, T.R.O.; Zefa, E.; Toma, G.A.; Cioffi, M.d.B.; de Oliveira, E.H.C.; O’Connor, R.E.; et al. Understanding the chromosomal evolution in cuckoos (Aves, Cuculiformes): A journey through unusual rearrangements. Genome 2024, 67, 168–177. [Google Scholar] [CrossRef] [Scilit]
  200. Kretschmer, R.; Gunski, R.J.; Garnero, A.d.V.; de Freitas, T.R.O.; Toma, G.A.; Cioffi, M.d.B.; de Oliveira, E.H.C.; O’Connor, R.E.; Griffin, D.K. Chromosomal analysis in Crotophaga ani (Aves, Cuculiformes) reveals extensive genomic reorganization and an unusual Z-autosome Robertsonian translocation. Cells 2020, 10, 4. [Google Scholar] [CrossRef] [Scilit]
  201. Nanda, I.; Schlegelmilch, K.; Haaf, T.; Schartl, M.; Schmid, M. Synteny conservation of the Z chromosome in 14 avian species (11 families) supports a role for Z dosage in avian sex determination. Cytogenet. Genome Res. 2008, 122, 150–156. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  202. Enguito, M.R.C.; Garnero, A.D.V.; Gunski, R.J.; de Souza, M.S.; O’Connor, R.E.; Srikulnath, K.; Singchat, W.; de Oliveira, E.H.C.; Romanov, M.N.; Griffin, D.K.; et al. Comparative chromosomal analysis of the Z chromosome in South American bird species shows a high rate of intrachromosomal rearrangements. Genes 2026, 17, 112. [Google Scholar] [CrossRef] [Scilit]
  203. Gunski, R.J.; Delgado Cañedo, A.; Garnero, A.d.V.; Ledesma, M.A.; Coria, N.; Montalti, D.; Degrandi, T.M. Multiple sex chromosome system in penguins (Pygoscelis, Spheniscidae). Comp. Cytogenet. 2017, 11, 541–552. [Google Scholar] [CrossRef] [Scilit]
  204. Sigeman, H.; Ponnikas, S.; Hansson, B. Whole-genome analysis across 10 songbird families within Sylvioidea reveals a novel autosome–sex chromosome fusion. Biol. Lett. 2020, 16, 20200082. [Google Scholar] [CrossRef] [Scilit]
  205. Pozzobon, L.C.; Toma, G.A.; Cioffi, M.d.B.; de Oliveira, E.H.C.; Kretschmer, R.; de Freitas, T.R.O. Karyotype evolution of Suliformes and description of a ♂Z1Z1Z2Z2/♀Z1Z2W multiple sex chromosome system in boobies (Sula spp.). Genome 2025, 68, 1–11. [Google Scholar] [CrossRef] [Scilit]
  206. Burley, J.T.; Orzechowski, S.C.M.; Sin, S.Y.W.; Edwards, S.V. Whole-genome phylogeography of the blue-faced honeyeater (Entomyzon cyanotis) and discovery and characterization of a neo-Z chromosome. Mol. Ecol. 2023, 32, 1248–1270. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  207. Muirhead, C.A.; Martí, E.; Shogren, E.H.; Uy, J.A.C.; Presgraves, D.C. Genomic origins and evolution of neo-sex chromosomes in Pacific island birds. Proc. Natl. Acad. Sci. USA 2025, 122, e2503746122. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  208. Griffin, D.K.; Kretschmer, R.; Larkin, D.M.; Srikulnath, K.; Singchat, W.; O’Connor, R.E.; Romanov, M.N. Did the evolution of multiple microchromosomes help save bird and other dinosaurs from extinction? Dev. Biol. 2026, 533, 89–111. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Contemporary avian phylogenetic tree and overview of the chromosomal changes that have occurred throughout evolution. Phylogenetic tree based on refs. [3,4] with all other artwork de novo by the authors. Orders where the “chicken-like” ancestral karyotype is largely retained are indicated alongside examples of rapid fission, fusion and inversion. The convergent chromosome 4 (present in chicken (Gallus gallus, Galliformes)) is noted, as are specific changes pertaining to the sex chromosomes.
Encyclopedia 06 00130 g001
Figure 2. Karyotype of the southern lapwing (Vanellus chilensis, Charadriiformes). On first inspection, this is similar to most birds including the one most studied—chicken (Gallus gallus, Galliformes). The ZZ chromosomes indicate that it is a male. A scale bar for 5 µm is provided.
Encyclopedia 06 00130 g002
Figure 3. Fluorescence in situ hybridization (FISH) on avian chromosomes, the technique on which most comparative and evolutionary studies have been based. (A) Whole chromosome probe derived from chicken (Gallus gallus, Galliformes) chromosome 1 (GGA1) and (B) white hawk (Leucopternis albicollis, Accipitriformes) chromosome 20 (LAL20) hybridized onto southern lapwing (Vanellus chilensis, Charadriiformes) chromosomes. (C) Identification of chicken microchromosome 26 ortholog (GGA26) by dual-color FISH using BAC (bacterial artificial chromosome) probes in V. chilensis chromosomes. The BACs used were CH261-186M13 (green) and CH261-170L23 (red). A scale bar for 5 µm is shown in the lower right corner of the micrographs.
Encyclopedia 06 00130 g003
Figure 4. Summary visualization of rearrangements of avian ancestral (AVI) chromosomes in chromosomes of reconstructed ancestors, extant descendants and outgroup species based on whole genome assemblies. Solid red-brown squares indicate avian chromosomes that were maintained as a single synteny block (either as a single chromosome or attached to another AVI chromosome), with shades of the color indicating the fraction of the chromosome affected by intrachromosomal rearrangements (lightest shade is most affected). Split blocks indicate which avian chromosomes were impacted by interchromosomal rearrangements. The percentage of the chromosome affected by extra intrachromosomal rearrangements is represented by upper triangles, whereas the fraction affected by interchromosomal modifications is represented by lower triangles. Acronyms for names of reconstructed ancestors correspond to the following: NEO, Neognathae; NEA, Neoaves; TAG, Telluraves and Aequornithia and Gruae; TAE, Telluraves and Aequornithia; TEL, Telluraves; EUF, Eufalconimorphae; PSI, Psittacopasserae; PAE, Passeriformes; PAR, Passeri; PPA, Passeroidea and Paroidea; PAO, Passeroidea; ETF, Estrildidae and Thraupidae and Fringillidae. Reprinted from Damas et al. [101].
Encyclopedia 06 00130 g004
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.