Perspective

Planetary Aerobiomes in Dust- and Aerosol-Dominated Extraterrestrial Environments

1
Department of Science and Technology, Parthenope University of Naples, 80143 Naples, Italy
2
INAF-OACN—Capodimonte Astronomical Observatory, 80131 Naples, Italy
3
CNR-IPCF—Institute for Chemical and Physical Processes, 98158 Messina, Italy
4
Department of Environmental Sciences, Informatics and Statistics, University of Venice Ca’ Foscari, 30123 Venice, Italy
*
Author to whom correspondence should be addressed.
Appl. Microbiol. 2026, 6(6), 66; https://doi.org/10.3390/applmicrobiol6060066
Submission received: 29 April 2026 / Revised: 27 May 2026 / Accepted: 28 May 2026 / Published: 30 May 2026

Abstract

The search for extraterrestrial life has traditionally focused on environments where liquid H2O is stable over long timescales, such as subsurface aquifers, hydrothermal systems, or ice-rich deposits. However, many planetary bodies are characterized by active cycles of particulate transport involving either mineral dust or atmospheric aerosols. In planetary science, these are commonly distinguished as refractory particles (non-volatile mineral dust) and volatile or mixed aerosol particles, including condensates such as ices, organics, or acidic droplets. Here, we propose the concept of planetary aerobiomes, defined as distributed particle-associated microbial persistence and dispersal systems in extraterrestrial environments. In this framework, refractory mineral particles may act as mobile particle-associated microenvironments that could support microbial survival and dispersal, while in some cases also providing partial physical shielding from environmental stressors. Drawing on observations from terrestrial dust-associated microbiomes and mineral–microbe interactions, particle-associated systems may represent previously overlooked ecological substrates in planetary environments. Rather than replacing models centred on environments with persistent liquid H2O, this perspective expands them by considering particle-associated microenvironments as transient but potentially relevant biosignature-preservation niches in arid, dust-dominated worlds such as Mars, as well as in aerosol-rich environments including Titan, Venus, and icy moons. We further discuss the implications for life-detection strategies, highlighting atmospheric particles as potential reservoirs of biosignatures, and consider their relevance for applied microbiology, including in situ resource utilization (ISRU) and bioregenerative life-support systems (BLSS). Beyond astrobiological implications, understanding microbial persistence within particle-associated extreme environments may provide useful models for applied microbiology, including stress-resilient microbial engineering, biomining, contamination control, and bioregenerative technologies for space exploration.

1. Introduction

Microorganisms associated with airborne particles represent an important topic in environmental and applied microbiology since atmospheric transport strongly influences microbial dispersal, persistence, and stress adaptation under extreme physicochemical conditions [1]. Studies of terrestrial bioaerosols have shown that microorganisms associated with mineral dust, volcanic ash, sea spray aerosols, and other particulates can tolerate desiccation, UV exposure, oxidative stress, nutrient limitation, and prolonged atmospheric transport [2]. These particle-associated microbial systems are relevant not only for microbial ecology and biogeochemical cycling, but also for biotechnology, contamination control, and planetary protection research. On Earth, atmospheric microbial communities are not only transported passively but can retain biological integrity during atmospheric residence [3]. Culture-dependent and culture-independent studies have detected bacteria, archaea, fungi, spores, ribosomes, nucleic acids, pigments, and stress-response signatures in aerosols, desert dust, marine spray, clouds, and high-altitude atmospheric samples [4]. These observations indicate that at least a subset of airborne microorganisms can remain viable or physiologically preserved during transport [4]. However, evidence for sustained cell division and population increase while suspended in air remains limited.
The search for life beyond Earth has long focused on the environmental niches where liquid H2O may persist for extended periods, including subsurface aquifers, hydrothermal systems, and ice-rich environments [5]. These systems can be considered among the most promising environments for preserving biosignatures, providing stable physicochemical conditions and long-term access to H2O, CNOPHS, and nutrients. Planetary life-detection strategies have mostly targeted sedimentary rocks, e.g., CO32−-bearing sandstones, SO42−-rich mudstones, conglomerates, and shales, subsurface ice, and aqueous mineral deposits, where biosignatures may accumulate and be preserved over geological timescales [6]. This paradigm is influenced by terrestrial models of microbial habitability and biosignature preservation. On Earth, microbial ecosystems are associated with environments where liquid H2O is abundant or periodically available, e.g., marine sediments, groundwater reservoirs, and permafrost [7]. These systems support continuous or episodic microbial metabolism and allow the formation of biological signatures such as organic molecules, microbially induced mineral structures, e.g., dubio-fossils and biominerals, and altered isotopic fractionation [8]. Several celestial bodies in the Solar System are characterized by particulate materials, including refractory mineral dust and volatile or mixed aerosol particles, that are mobilized by atmospheric or surface processes rather than by stable aqueous systems [9]. On Mars, global and regional dust storms inject large quantities of micron-scale refractory mineral particles into the atmosphere and redistribute them across the entire planet [10]. These processes generate a highly dynamic surface-atmosphere system in which particles are continuously transported, deposited, and resuspended. However, the intense UV radiation, oxidizing surface chemistry, and extreme desiccation conditions are expected to severely limit long-term microbial survival in exposed environments. In this context, the potential role of refractory dust particles is not to sustain active microbial ecosystems but rather to act as transient carriers and microenvironments that may allow the transport and temporary persistence of dormant microorganisms, particularly within shielded niches such as mineral microfractures or particle aggregates. Comparable particle-rich atmospheric environments also exist elsewhere in the Solar System, including the dense organic haze layers of Titan and the aerosol clouds of Venus [11].
Atmospheric particles, including both refractory dust and aerosol particles, have received limited attention as potential microbial habitats and biosignature-hosting environments, both on Earth and in extraterrestrial settings [12]. Microorganisms associated with desert dust, volcanic ash, and marine aerosols, including members of the Actinobacteria, Bacteroidetes, Proteobacteria, Firmicutes, and cyanobacteria, have been shown to remain viable after intercontinental dispersal, demonstrating tolerance to desiccation, radiation, temperature fluctuations, and nutrient limitation [13]. In addition, Archaea, including chemolithoautotrophic ammonia oxidisers, and fungi belonging to genera such as Alternaria, Aspergillus, Cladosporium, and Penicillium have been detected in sandstorms [13]. This suggests that atmospheric particles, particularly refractory mineral dust in dust-dominated environments, may function as microhabitats for microbial survival and dispersal. Even under extremely dry conditions, mineral surfaces can adsorb films of H2O and concentrate trace nutrients or redox-active compounds, e.g., biometals [14,15]. Such micro-environments may support the temporary persistence of dormant microorganisms and, under transiently favorable conditions, limited metabolic maintenance or cellular repair. In this context, refractory dust particles may act not as passive transport vectors but as potential ecological substrates under favourable micro-environmental conditions. Terrestrial aero-microbiology should not be directly extrapolated to extraterrestrial environments without considering major physicochemical constraints. Although airborne microorganisms on Earth can retain viability and, in some cases, limited metabolic activity [16], current evidence does not demonstrate sustained cell division or long-term population growth while suspended in atmospheric particles. Most experimental support derives from laboratory simulations or terrestrial analogue environments. Consequently, extraterrestrial particle-associated microbial systems are more appropriately discussed in terms of persistence, dormancy, dispersal, biosignature preservation, and transient metabolic activation rather than stable atmospheric ecosystems.
Here, we propose the concept of planetary aerobiomes as particle-associated microbial persistence and dispersal frameworks linked to atmospheric particles in extraterrestrial environments, i.e., refractory dust and aerosol particles, on other celestial bodies. Unlike conventional ecosystems confined to stable habitats, aerobiomes would represent distributed and dynamic particle-associated microbial systems shaped by atmospheric circulation and particle transport. Active microbial growth is not assumed within this framework and would require independent evidence for sufficient H2O activity, compatible temperature ranges, redox disequilibrium, radiation tolerance, and residence times compatible with cellular processes. In this framework, inclusion within a planetary aerobiome requires: (i) the presence of mobilizable atmospheric or surface-derived particles; (ii) a mechanism for microbial attachment or persistence; and (iii) environmental conditions capable of supporting at least transient biological stability or biosignature preservation.
If microbial life can persist in association with atmospheric particles, including refractory dust and volatile or mixed aerosol particles, these may represent previously overlooked targets for life-detection strategies in space. Microorganisms capable of surviving within such extreme environments may possess metabolic and physiological traits relevant for space biotechnology and astrobiology, including in situ resource utilization (ISRU) [17,18].

2. Refractory Dust as a Potential Microbial Microenvironment

Refractory mineral dust particles possess several physicochemical properties that pose them as suitable microhabitats. Under dry conditions, minerals can adsorb H2O from the atmosphere via hygroscopic adsorption and capillary condensation [19]. Laboratory studies and observations from terrestrial deserts have shown that microscopic H2O films associated with mineral grains can persist in the absence of bulk liquid H2O [14]. Beyond H2O adsorption, dust particles exhibit complex mineralogical compositions, including calcite (CaCO3), gypsum (CaSO4), quartz (SiO2), plagioclase [(Na, Ca)(Si, Al)4O8], and K-feldspar (KAlSi3O8), which generate localized geochemical gradients [20]. Many planetary regoliths contain Fe-bearing minerals (hematite-Fe2O3), sulfides (pyrite-FeS2), silicates [olivine-(Mg,Fe)2SiO4], and other redox-active minerals, e.g., jarosite-KFe2(SO4)2(OH)6, that may participate in localized redox interactions potentially relevant to lithotrophic and other extremophilic microorganisms [21]. In terrestrial environments, a wide range of microorganisms, e.g., Acidithiobacillus, Sphingomonas, Cupriavidus genera, colonize mineral surfaces and exploit redox reactions involving elements such as Fe, Cu, S, or Mn, Ce [18,22,23]. In terrestrial environments, these metabolisms allow microorganisms to exploit mineral-associated redox gradients independently of organic C sources.
The nano-to-micrometre-scale size, irregular morphology, mineralogical heterogeneity, and chemical composition of refractory dust particles may further enhance their ecological potential. Surface irregularities, micro-to-nano-fractures, and mineral inclusions within individual particles can create microscale redox gradients, hydration–dehydration phenomena, and localized shielding from radiation [24]. Fractures can also concentrate nutrients and provide localized shielding from environmental stressors [24]. In terrestrial mineral–microbe interactions, microbial colonization often occurs preferentially along mineral boundaries, pores, or fracture surfaces [25]. These physicochemical and ecological niches suggest that refractory mineral dust particles may represent potential ecological reservoirs for dormant microorganisms and, possibly for transient metabolic maintenance or cellular repair under short-lived favorable conditions.

3. The Planetary Aerobiome Concept

The planetary aerobiome concept extends terrestrial observations to extraterrestrial environments by proposing that atmospheric particles, i.e., a broad category encompassing refractory mineral dust particles, organic aerosol particles, sulfuric-acid droplets, and ice grains generated or transported by planetary atmospheric or plume-related processes, could form distributed particle-associated microbial persistence and dispersal systems (Figure 1). In such systems, microorganisms would not be confined to stable habitats but would be associated with atmospheric particles that are continuously mobilized or transported by atmospheric circulation. Atmospheric particles could therefore function as ecological substrates and dispersal vectors, linking surface environments with atmospheric transport processes. Microorganisms associated with these particles could be lifted, transported, and redeposited by atmospheric processes, generating a highly mobile particle-associated microbial dispersal system capable of dispersing across large planetary distances as suggested by the recovery of microbial spores from stratospheric dust particles [26]. Such systems would operate on spatial scales far exceeding those of most terrestrial microbial ecosystems, allowing microorganisms or dormant propagules to disperse across separated regions through repeated cycles of atmospheric transport. Environmental conditions on many planetary surfaces, including Mars, are unlikely to support sustained metabolic activity in most microorganisms [27]. Although stable liquid H2O is unlikely within suspended Martian dust particles under present atmospheric conditions, hygroscopic salt phases, deliquescence phenomena, and temporary fluctuations in atmospheric humidity may permit limited adsorption of H2O molecules or the formation of microscale hydrated films on mineral particles under highly localized and transient conditions [28]. Such processes could contribute to molecular stabilization and biosignature preservation in dormant microorganisms, including highly desiccation-tolerant taxa such as Halomonas spp. and Marinococcus spp., rather than sustained metabolic activity or growth [29].
The particle-associated microbial system would therefore be characterized not by localized and persistent microbial communities, but by a distributed and transient ecological network in which microorganisms are associated with, and transported by, atmospheric particles through repeated cycles of entrainment, transport, and surface deposition. A planetary aerobiome thus represents a fundamentally different ecological architecture, shaped by atmospheric dynamics, particle–microbe interactions, and extreme environmental variability. The potential existence of planetary aerobiomes is strongly constrained by environmental factors including H2O activity, UV and ionizing radiation, oxidizing chemistry, ClO4 presence, acidity, ionic strength, temperature, and residence time in suspension. On Mars, low H2O activity, oxidants, UV radiation, and repeated desiccation restrict most particle-associated microorganisms to dormant persistence or transient repair processes [30]. In Venusian aerosols, concentrated H2SO4 droplets and extremely low H2O activity represent barriers for cellular maintenance and growth [31]. Titan’s cryogenic temperatures impose severe kinetic limitations on Earth-like biochemistry despite the abundance of atmospheric organic aerosols [32]. Consequently, the planetary aerobiome concept should primarily be interpreted as a framework for evaluating particle-associated microbial persistence, dispersal, and biosignature preservation under different planetary conditions.

4. Relevance to Planetary Environments

The aerobiome concept is particularly relevant to planetary environments where fine-grained surface materials are readily mobilized into atmospheric particles, dominating surface-to-atmosphere interactions (Table 1) [33].

4.1. Mars

The Martian surface is covered by extensive deposits of fine-grained regolith, including dust fractions typically in the micrometre range, that are readily mobilized by wind-driven processes [34]. Regional and global dust storms inject large quantities of micron-scale refractory dust particles into the atmosphere [35], where they remain suspended for extended periods before settling back onto the surface. These processes create a dynamic surface-atmosphere system characterized by continuous cycles of particle lifting, transport, and deposition. If microorganisms, or biosignatures, were present within the Martian regolith, dust storms could redistribute them across vast planetary distances. This mechanism would allow microbial populations to be redistributed across geographically distant regions, maintaining potential connectivity between otherwise isolated habitats.
Martian dust contains Fe-bearing minerals, sulfates, silicates, and other redox-active mineral phases, e.g., gypsum, jarosite [KFe3(SO4)2(OH)6], goethite [α-Fe3+O(OH)], and hematite (Fe2O3), that could interact with lithotrophic metabolisms under localized and highly constrained conditions [36]. However, many of these minerals are already oxidized due to prolonged surface exposure and small particle size, potentially limiting the energetic feasibility of oxidative lithotrophic pathways within suspended particulate environments [37]. Potential metabolisms would involve localized redox disequilibria associated with reduced trace mineral phases, regolith microenvironments, or interactions with atmospheric gases such as CO or trace CH4 [38], rather than sustained energy generation within airborne dust particles [39]. Although hydration events, if they occur, would be brief and spatially restricted, they may contribute to temporary molecular stabilization, limited cellular repair, or biosignature preservation within particle-associated microenvironments [40]. Under present Martian atmospheric conditions, refractory dust particles are more plausibly interpreted as transient transport and preservation media rather than extreme environments capable of supporting sustained microbial activity.

4.2. Titan

Titan is the largest moon of Saturn and represents another environment where atmospheric particles dominate planetary chemistry [35]. Titan is characterized by a dense N-rich atmosphere containing complex organic aerosols commonly referred to as tholins (CXHYNZ) [41]. These particles form extensive haze layers that shape Titan’s atmospheric dynamics and surface chemistry.
Although Titan’s extremely low temperatures impose severe constraints on conventional biological processes, aerosol particles may nonetheless represent chemically rich environments in which complex organic compounds accumulate [42]. Any hypothetical particle-associated biological system on Titan would require metabolic biochemical strategies adapted to Titan’s cryogenic conditions. While the possibility of life in Titan’s atmosphere remains speculative, the presence of abundant aerosol particles suggests that particle-associated ecological structures may instead represent a speculative boundary case for evaluating particle-associated habitability and biosignature preservation under cryogenic conditions [42].

4.3. Venus

The cloud layers of Venus consist of dense acid aerosol droplets primarily composed of H2SO4 solutions, suspended within a thick CO2 atmosphere [43]. These cloud particles dominate the planet’s atmospheric chemistry and may remain stable within certain altitude ranges for extended periods [43].
Some studies have suggested that microbial life could potentially survive within the temperate regions of Venus’ cloud layers, where temperatures and pressures are less extreme than at the surface. For example, the lower cloud region has a temperature of 60 °C and a pressure of 1 atm [44]. If microorganisms can tolerate the acidity of Venusian clouds, acid aerosol droplets could represent microhabitats analogous to those proposed in the aerobiome concept. In such a scenario, microbial cells would be associated with aerosol particles and dispersed through atmospheric circulation, forming a hypothetical particle-associated ecosystem suspended within the acidic cloud layers and supporting C fixation pathways based on CO2.

4.4. Icy Moons

Unlike Mars, Venus, or Titan, the astrobiological relevance of icy moons, e.g., Europa, Ganymede, Callisto, and Enceladus, is linked to subsurface ocean environments rather than atmospheric particle systems. Several moons of Jupiter and Saturn are believed to host subsurface oceans beneath thick ice shells [45]. In these systems, surface ice is continuously processed by radiation, micrometeorite impacts, and tectonic or cryovolcanic activity, generating fine-grained ice particles that may be transported across the surface or ejected into space [46].
On Europa, energetic particle irradiation from Jupiter’s magnetosphere alters the chemistry of the surface ice, producing oxidants and other reactive compounds that may accumulate within the upper layers of the ice shell [47]. Mechanical fracturing and resurfacing processes generate ice grains and particulate material that can be redistributed across the moon’s surface. If material from the subsurface ocean is transported upward through fractures or plume activity, these particles may incorporate ocean-derived salts, organic molecules, or potentially microbial cells. Similarly, Enceladus exhibits cryovolcanic plume activity at its south pole, sourced by a subsurface ocean influenced by hydrothermal water–rock interactions [47].
Although the physical conditions of icy moons differ substantially from those of dust-dominated planetary atmospheres, particle-associated processes may still play an important ecological and biochemical role. Ice grains or frost particles could act as carriers that concentrate organic molecules, salts, and other chemical species originating from subsurface oceans. In this context, icy moons may host cryogenic aerobiome-like systems, in which particle transport processes link subsurface aquatic habitats with surface or atmospheric environments. In this context, icy moons are included primarily because particle transport processes may connect subsurface habitats with accessible surface or plume materials relevant to biosignature sampling.

5. Physicochemical Constraints on Planetary Aerobiomes and Microbial Stress-Response Strategies

Any planetary aerobiome framework must be evaluated against the physicochemical constraints that limit microbial survival and activity in extraterrestrial particulate environments. The persistence of microorganisms within atmospheric particles depends not only on transport processes and mineral microenvironments, but also on the capacity of cells to tolerate extreme desiccation, low H2O activity, oxidizing chemistry, UV and ionizing radiation, temperature fluctuations, acidity, ionic stress, and prolonged nutrient limitation. In most extraterrestrial environments, these factors are expected to constrain sustained microbial growth and restrict particle-associated systems to dormant persistence, biosignature preservation, transient metabolic maintenance, or short-lived repair processes.
Among these constraints, H2O activity represents one of the most critical parameters controlling microbial viability [48]. On Mars, atmospheric relative humidity is low and transient liquid H2O is thought to occur mainly as highly saline brines enriched in ClO4 and SO42− [28]. Such environments may exhibit H2O activities below the accepted limit for active terrestrial microbial growth (~0.585 aw) [49]. Several terrestrial extremophiles possess physiological adaptations that permit persistence under severe desiccation and osmotic stress [50]. Members of the genera Halomonas, Marinococcus, and Deinococcus accumulate solutes such as ectoine, hydroxyectoine, trehalose, glycine betaine, and proline to maintain osmotic balance and stabilize proteins and membranes during dehydration-rehydration cycles [51]. In particular, ectoine biosynthesis, mediated by the ectABC gene cluster, plays a central role in halotolerance and desiccation resistance in halophilic and halotolerant bacteria [52]. Trehalose accumulation additionally contributes to membrane stabilization and vitrification processes during extreme dehydration [53].
Desiccation is associated with oxidative stress because it promotes protein denaturation, membrane destabilization, and intracellular reactive oxygen species (ROS) accumulation [54]. To avoid these effects, extremophiles express antioxidant enzymes including catalase, superoxide dismutase (SOD), peroxidases, and thioredoxin-dependent systems [55]. Deinococcus radiodurans, used as a model organism for radiation and desiccation resistance, combines efficient antioxidant defenses with DNA repair capacity [55]. This microorganism possesses multiple genome copies, Mn-dependent antioxidant complexes, and DNA repair pathways involving RecA-mediated homologous recombination, extended synthesis-dependent strand annealing, DNA ligases, and DNA damage response proteins such as PprA [55]. Similar stress-response mechanisms are observed in Bacillus spores, which combine metabolic dormancy, DNA-binding small acid-soluble proteins (SASPs), dipicolinic acid accumulation, and multilayered spore envelopes to tolerate UV irradiation, oxidation, and prolonged desiccation [56].
Radiation exposure represents another challenge for hypothetical planetary aerobiomes. On Mars, the absence of a global magnetic field and the thin atmosphere expose surface particles to ultraviolet radiation and ionizing cosmic radiation [57]. UV-C radiation in particular can induce pyrimidine dimers, DNA strand breaks, membrane oxidation, and protein damage [58]. Several terrestrial microorganisms mitigate UV stress through pigment production, biofilm formation, and DNA repair mechanisms. Pigmented microorganisms such as Chroococcidiopsis spp. and certain Actinobacteria synthesize carotenoids, scytonemin, and melanin-like compounds that absorb radiation and reduce oxidative damage [59]. Additional protection may derive from particle-associated shielding, mineral inclusions, and aggregation within biofilms or dust clusters. Biofilm-associated extracellular polymeric substances (EPS) can reduce H2O loss, adsorb ions, trap nutrients, and attenuate radiation penetration [60]. EPS matrices also facilitate adhesion to mineral surfaces and may enhance microbial persistence within pores, fractures, or particle aggregates.
The oxidizing geochemistry of extraterrestrial environments constitutes an additional limitation. Martian regolith contains ClO4, Fe oxides, sulfates, and reactive oxidants capable of generating severe oxidative stress and damaging biomolecules [61]. Although ClO4 are often considered inhibitory to life, some terrestrial microorganisms possess metabolic or physiological adaptations that permit tolerance or utilization of these compounds. Perchlorate-reducing bacteria such as Dechloromonas, Azospira, and Magnetospirillum species express ClO4 reductase and ClO2 dismutase enzymes, enabling the reduction of ClO4 to Cl and O2 [62]. While such metabolisms require liquid H2O and suitable redox conditions unlikely to be widespread on the Martian surface, they demonstrate that oxidant-rich environments are not universally incompatible with microbial survival. Fe- and S-metabolizing microorganisms including Acidithiobacillus ferrooxidans and Sulfobacillus spp. additionally illustrate how lithotrophic metabolisms may exploit redox-active mineral phases under highly oligotrophic conditions [18].
Venusian aerosols introduce additional challenges related to H2SO4 exposure and extremely low H2O activity. Concentrated H2SO4 droplets are expected to denature biomolecules, destabilize membranes, and disrupt H+ gradients essential for cellular energetics [31]. Terrestrial acidophiles such as A. ferrooxidans, Ferroplasma acidiphilum, and Acidiphilium spp. survive under low pH conditions by maintaining steep proton gradients across the membrane, expressing acid-stable proteins, and modifying membrane lipid composition to reduce proton permeability [63]. However, current evidence suggests that the combined acidity and H2O activity conditions proposed for Venusian cloud droplets exceed the tolerance limits of known terrestrial microorganisms [44]. Venus should presently be regarded as a highly speculative boundary case for particle-associated habitability.
Cryogenic temperatures on Titan similarly impose severe kinetic and thermodynamic limitations on Earth-like metabolism. Low temperatures reduce enzymatic reaction rates, membrane fluidity, nutrient diffusion, and intracellular transport processes [64]. Psychrophilic microorganisms on Earth partially mitigate these effects through cold-adapted enzymes, unsaturated membrane lipids, antifreeze proteins, and cryoprotectants such as trehalose and exopolysaccharides [64]. Titan’s environmental conditions remain far beyond the physiological range of known terrestrial aerosol microbiology. In this context, Titan is more plausibly interpreted as a chemically relevant environment for organic aerosol accumulation and biosignature preservation rather than as a site of active particle-associated microbial ecosystems [65].
These observations suggest that the most plausible interpretation of planetary aerobiomes is not that of continuously active atmospheric biospheres, but rather of constrained particle-associated systems in which microorganisms, if present, would rely on dormancy, stress-response pathways, mineral shielding, transient hydration events, and efficient molecular repair mechanisms to persist under extreme environmental conditions.

6. Implications for Life-Detection Strategies

Recognizing the possibility of planetary aerobiomes may have significant implications for the design of future life-detection missions and for present missions such as ESA-JUICE and NASA Europa Clipper. If microbial material, dormant cells, or biosignatures can persist in association with atmospheric particles, including refractory dust, biosignatures may not be confined to rocks, sediments, or subsurface reservoirs but could be present within mobile particulate material (Table 2). Most current life-detection approaches are largely motivated by the expectation that biosignatures accumulate and are preserved within mineral matrices over long timescales. Consequently, planetary missions have prioritized the analysis of sedimentary rocks, hydrated minerals, ice deposits, or subsurface environments where traces of past or present biological activity may be concentrated [66].
Here, we suggest that atmospheric particles and their surface deposits could serve as targets for astrobiological investigation. Sampling atmospheric or suspended particulate material may provide access to spatially integrated biosignatures and organic material derived from multiple geological environments and transport pathways. Atmospheric particles are unlikely to contain biosignatures distinct from those preserved in rocks, sediments, evaporites, or ice deposits. However, particulate sampling may provide complementary access to mobile material integrating signals from multiple source regions that may be difficult to investigate through localized surface analyses alone. If microbial cells (or dormant propagules) are present within the regolith, atmospheric transport may increase the likelihood that they are encountered by surface instruments. Incorporating atmospheric particle sampling into life-detection strategies may therefore broaden the range of environments investigated in the search for extraterrestrial life.
Future missions could incorporate dedicated systems for collection and analysis of atmospheric particles, including refractory dust and aerosol particles. Landers or rovers equipped with electrostatic collectors or filtration devices (such as the one shown in [26]), may capture particulate material during wind events or dust storms, allowing the accumulation of sufficient samples for subsequent investigation. Once collected, particulate samples could be examined using microscopic imaging techniques, e.g., Scanning Electron Microscopy-SEM, to identify potential morphological biosignatures such as cell-like structures, microbial aggregates, or characteristic mineral-to-organic associations [67]. Complementary analytical approaches may include spectroscopic detection of organic molecules, lipid fragments, or isotopic fractionation patterns that could indicate biological activity or preserved biomolecules. Atmospheric particle sampling may additionally represent a comparatively low-mass and operationally flexible strategy for preliminary environmental screening and broad regional biosignature surveys during future planetary missions. Different missions, such as DUSTER (Dust in the Upper Stratosphere Tracking Experiment and Retrieval) already show an easy and costless way to sample stratospheric particulates in terrestrial environments [26].

7. Implications for Applied Microbiology and Space Biotechnology

From an applied microbiology perspective, the planetary aerobiome framework is relevant because it focuses attention on microbial survival strategies under aerosolized, desiccated, irradiated, and mineral-rich conditions. Understanding how microorganisms tolerate particle-associated environmental stress may support the development of robust microbial systems for space biotechnology, contamination control, environmental management, and planetary protection applications. Stress-tolerance mechanisms are characteristic of several terrestrial extremophilic and polyextremophilic microorganisms associated with mineral-rich and desiccating environments [68]. Relevant adaptive traits include sporulation, metabolic downregulation, antioxidant systems, DNA repair pathways, EPS, mineral adhesion, and biofilm-associated protection. Such traits are observed in several terrestrial extremophiles, including members of the genera Deinococcus and Gemmatimonas, which may represent valuable biological resources for biotechnology in extraterrestrial environments where conventional microbial processes are difficult to sustain [69]. Beyond survival, these physiological capabilities may also support metabolically active processes relevant to resource utilization and environmental engineering in extraterrestrial systems. Microorganisms adapted to mineral substrates may play a key role in in situ resource utilization (ISRU) strategies aimed at converting planetary materials into usable resources [17,22]. Lithotrophic microorganisms, such as those belonging to the Acidithiobacillus genus, are capable of deriving energy from mineral redox reactions, which could potentially facilitate processes such as mineral weathering, biomining, or the mobilization of essential nutrients from planetary regolith [18]. These processes may enable the biological extraction of elements required for life support systems, including Fe, S, P, or trace metals, while simultaneously contributing to the transformation of raw geological materials into biologically accessible substrates [18,22].
Understanding how living organisms persist and function in particle-rich environments may also inform the design of BLSS for long-duration space missions and extraterrestrial habitats [70]. Microbial communities capable of operating under conditions of limited H2O availability, low nutrient fluxes, and high environmental variability provide platforms for waste recycling, resource recovery, and environmental stabilization [71]. From this perspective, the study of particle-associated microbial survival strategies may not only advance our understanding of potential extraterrestrial particle-associated microbial systems but also guide the development of microbial technologies capable of operating under the extreme constraints of space environments [72]. The study of microbial persistence on particulate materials is also relevant to contamination control and planetary protection. Dust and aerosol particles may facilitate the dispersal and persistence of terrestrial microorganisms within spacecraft-associated environments or after accidental release onto planetary surfaces. Investigating microbial attachment, survival, and inactivation on mineral particles may therefore improve sterilization protocols, bioburden monitoring, and life-detection strategies while reducing the risk that terrestrial contamination compromises the scientific integrity of astrobiological investigations [22].

8. Conclusions

Atmospheric particles, including refractory dust and aerosol particles, represent ubiquitous yet underexplored components of many planetary environments. By functioning as mobile micro-environments, these particles may contribute to microbial persistence, dispersal, biosignature preservation, and, under restrictive and transient conditions, limited metabolic maintenance. Refractory mineral grains, aerosol particles, and ice grains can concentrate H2O molecules, nutrients, organic compounds, and redox-active compounds while simultaneously offering partial protection from environmental stressors such as radiation and desiccation. As a result, particle-associated microenvironments may represent transient ecological niches even in planetary settings where H2O activity is low. The concept of planetary aerobiomes provides a new framework for considering how particle-associated microbial systems might persist under such extreme planetary conditions. Rather than being confined to stable aqueous habitats, particle-associated microbial systems may persist as distributed and transient networks maintained through cycles of atmospheric transport, deposition, and intermittent hydration. In this perspective, atmospheric dynamics become a component of planetary microbial ecology, linking surface mineral environments with atmospheric circulation and enabling microbial dispersal across planetary scales. Recognizing the potential role of particle-associated microbial persistence systems may therefore broaden current approaches to the search for extraterrestrial life. These particles may act not only as transport vectors but also as carriers of biosignatures, integrating biological material from multiple surface environments. Incorporating atmospheric particle sampling and analysis into future planetary missions could thus expand the range of accessible biosignatures and provide new opportunities for detecting evidence of past or present microbial activity. The planetary aerobiome concept should therefore be regarded as a cautious framework for investigating particle-associated microbial persistence and biosignature transport under extreme planetary conditions rather than as evidence for stable extraterrestrial atmospheric ecosystems.

Author Contributions

Conceptualization, L.T.; investigation, L.T.; writing—original draft preparation, L.T.; writing—review and editing, L.T., M.E., P.D.D. and A.R.; visualization, L.T. and M.E.; supervision, A.R.; project administration, A.R.; funding acquisition, P.D.D. and A.R. All authors have read and agreed to the published version of the manuscript.

Funding

This work has been conducted thanks to the following funding: the ASI-INAF agreements I/024/12/0 and 2020-4-HH.0 by the Italian Space Agency (ASI).

Institutional Review Board Statement

Not applicable.

Informed Consent Statement

Not applicable.

Data Availability Statement

No new data were created.

Acknowledgments

L.T. would like to express sincere gratitude to the DUSTER (Dust in the Upper Stratosphere Tracking Experiment and Retrieval) team and to the APCL (Astrobiology and Cosmic Physics Laboratory) of the Parthenope University of Naples for the valuable discussions that contributed to the development of the idea of an extraterrestrial planetary aerobiome. L.T. is also grateful to the “dust” research teams of INAF-OACN (Astronomical Observatory of Capodimonte, Naples, Italy), CNR-IPCF (Institute for Chemical-Physical Processes, Messina, Italy), and University of Pisa, for their invaluable support and for sharing their deep knowledge of the fascinating world of cosmic dust and, more broadly, dust environments.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Šantl-Temkiv, T.; Amato, P.; Casamayor, E.O.; Lee, P.K.H.; Pointing, S.B. Microbial ecology of the atmosphere. FEMS Microbiol. Rev. 2022, 46, fuac009. [Google Scholar] [CrossRef] [Scilit]
  2. Griffin, D.W. Atmospheric Movement of Microorganisms in Clouds of Desert Dust and Implications for Human Health. Clin. Microbiol. Rev. 2007, 20, 459–477. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Amato, P.; Joly, M.; Besaury, L.; Oudart, A.; Taib, N.; Moné, A.I. Active microorganisms thrive among extremely diverse communities in cloud water. PLoS ONE 2017, 12, e0182869. [Google Scholar] [CrossRef] [Scilit]
  4. Després, V.R.; Huffman, J.A.; Burrows, S.M.; Hoose, C.; Safatov, A.S.; Buryak, G.; Fröhlich-Nowoisky, J.; Elbert, W.; Andreae, M.; Pöschl, U.; et al. Primary biological aerosol particles in the atmosphere: A review. Tellus B Chem. Phys. Meteorol. 2012, 64, 15598. [Google Scholar] [CrossRef] [Scilit]
  5. Vidal, E.; Lindsay, M.R.; Bradley, J.A.; Osburn, M.R.; Ruff, S.E. Subsurface Life on Earth as a Key to Unlock Extraterrestrial Mysteries. Microb. Biotechnol. 2025, 18, e70286. [Google Scholar] [CrossRef] [Scilit]
  6. Merino, N.; Aronson, H.S.; Bojanova, D.P.; Feyhl-Buska, J.; Wong, M.L.; Zhang, S. Living at the Extremes: Extremophiles and the Limits of Life in a Planetary Context. Front. Microbiol. 2019, 10, 447668. [Google Scholar] [CrossRef] [Scilit]
  7. Hallsworth, J.E. Water is a preservative of microbes. Microb. Biotechnol. 2022, 15, 191–214. [Google Scholar] [CrossRef] [Scilit]
  8. Orcutt, B.N.; LaRowe, D.E.; Biddle, J.F.; Colwell, F.S.; Glazer, B.T.; Reese, B.K.; Kirkpatrick, J.B.; Lapham, L.L.; Mills, H.J.; Sylvan, J.B.; et al. Microbial activity in the marine deep biosphere: Progress and prospects. Front. Microbiol. 2013, 4, 189. [Google Scholar] [CrossRef] [Scilit]
  9. Foucher, F.; Hickman-Lewis, K.; Hutzler, A.; Joy, K.H.; Folco, L.; Bridges, J.C.; Wozniakiewicz, P.; Martínez-Frías, J.; Debaille, V.; Zolensky, M.; et al. Definition and use of functional analogues in planetary exploration. Planet. Space Sci. 2021, 197, 105162. [Google Scholar] [CrossRef] [Scilit]
  10. Streeter, P.; Lewis, S.; Patel, M.; Holmes, J. Impacts of the 2018 Global Dust Storm on martian polar vortex dynamics. In Proceedings of the 14th Europlanet Science Congress 2020, Virtual Event, 21 September–9 October 2020; p. EPSC2020-894. [Google Scholar]
  11. Hörst, S.M. Titan’s atmosphere and climate. J. Geophys. Res. Plan. 2017, 122, 432–482. [Google Scholar] [CrossRef] [Scilit]
  12. Preston, L.J.; Dartnell, L.R. Planetary habitability: Lessons learned from terrestrial analogues. Int. J. Astrobiol. 2014, 13, 81–98. [Google Scholar] [CrossRef] [Scilit]
  13. Behzad, H.; Mineta, K.; Gojobori, T. Global Ramifications of Dust and Sandstorm Microbiota. Genome Biol. Evol. 2018, 10, 1970–1987. [Google Scholar] [CrossRef] [Scilit]
  14. Boxe, C.S.; Hand, K.P.; Nealson, K.H.; Yung, Y.L.; Yen, A.S.; Saiz-Lopez, A. Adsorbed water and thin liquid films on Mars. Int. J. Astrobiol. 2012, 11, 169–175. [Google Scholar] [CrossRef] [Scilit]
  15. Hay Mele, B.; Monticelli, M.; Leone, S.; Bastoni, D.; Barosa, B.; Cascone, M. Oxidoreductases and metal cofactors in the functioning of the earth. Essays Biochem. 2023, 67, 653–670. [Google Scholar] [CrossRef] [Scilit]
  16. Lappan, R.; Thakar, J.; Molares Moncayo, L.; Besser, A.; Bradley, J.A.; Goordial, J.; Trembath-Reichert, E.; Greening, C. The atmosphere: A transport medium or an active microbial ecosystem? ISME J. 2024, 18, wrae092. [Google Scholar] [CrossRef] [Scilit]
  17. Tonietti, L.; Barosa, B.; Pioltelli, E.; Giovannelli, D.; Covone, G.; Di Donato, P. Exploring the Development of Astrobiology Scientific Research through Bibliometric Network Analysis: A Focus on Biomining and Bioleaching. Minerals 2023, 13, 797. [Google Scholar] [CrossRef] [Scilit]
  18. Tonietti, L.; Esposito, M.; Cascone, M.; Barosa, B.; Fiscale, S.; Muscari Tomajoli, M.T. Unveiling the Bioleaching Versatility of Acidithiobacillus ferrooxidans. Microorganisms 2024, 12, 2407. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Yalcin, S.E.; Legg, B.A.; Yeşilbaş, M.; Malvankar, N.S.; Boily, J.-F. Direct observation of anisotropic growth of water films on minerals driven by defects and surface tension. Sci. Adv. 2020, 6, eaaz9708. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Jeong, G.Y. Mineralogy and geochemistry of Asian dust: Dependence on migration path, fractionation, and reactions with polluted air. Atmos. Chem. Phys. 2020, 20, 7411–7428. [Google Scholar] [CrossRef] [Scilit]
  21. Ramkissoon, N.K.; Pearson, V.K.; Schwenzer, S.P.; Schröder, C.; Kirnbauer, T.; Wood, D.; Seidel, R.G.; Miller, M.A.; Olsson-Francis, K. New simulants for martian regolith: Controlling iron variability. Planet. Space Sci. 2019, 179, 104722. [Google Scholar] [CrossRef] [Scilit]
  22. Tonietti, L.; Esposito, M.; Leggiero, M.; Bunn, F.; Eades, L.J.; Cordone, A.; Horsfall, L.; Covone, G.; Cockell, C.S.; Giovannelli, D.; et al. Bioleaching of critical trace metals by Sphingomonas desiccabilis: Substrate-driven selectivity in Earth and space analogues. Front. Microbiol. 2026, 17, 1741305. [Google Scholar] [CrossRef] [Scilit]
  23. Santomartino, R.; Blanco, G.R.; Gudgeon, A.; Hafner, J.; Stirpe, A.; Waterfall, M.; Cayzer, N.; Pichevin, L.; Calder, G.; Birkenfeld, K.R.; et al. Testing microbial biomining from asteroidal material onboard the International Space Station. npj Microgravity 2026, 12, 23. [Google Scholar] [CrossRef] [Scilit]
  24. Vogel, C.; Helfenstein, J.; Massey, M.S.; Sekine, R.; Kretzschmar, R.; Beiping, L.; Peter, T.; Chadwick, O.A.; Tamburini, F.; Rivard, C.; et al. Microspectroscopy reveals dust-derived apatite grains in acidic, highly-weathered Hawaiian soils. Geoderma 2021, 381, 114681. [Google Scholar] [CrossRef] [Scilit]
  25. Cockell, C.S.; Santomartino, R.; Finster, K.; Waajen, A.C.; Eades, L.J.; Moeller, R.; Rettberg, P.; Fuchs, F.M.; Van Houdt, R.; Leys, N.; et al. Space station biomining experiment demonstrates rare earth element extraction in microgravity and Mars gravity. Nat. Commun. 2020, 11, 5523. [Google Scholar] [CrossRef] [Scilit]
  26. Della Corte, V.; Rietmeijer, F.J.M.; Rotundi, A.; Ferrari, M. Introducing a new stratospheric dust-collecting system with potential use for upper atmospheric microbiology investigations. Astrobiology 2014, 14, 694–705. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Sielaff, A.C.; Smith, S.A. Habitability of Mars: How Welcoming Are the Surface and Subsurface to Life on the Red Planet? Geosciences 2019, 9, 361. [Google Scholar] [CrossRef] [Scilit]
  28. Martín-Torres, F.J.; Zorzano, M.-P.; Valentín-Serrano, P.; Harri, A.-M.; Genzer, M.; Kemppinen, O.; Rivera-Valentin, E.G.; Jun, I.; Wray, J.; Bo Madsen, M.; et al. Transient liquid water and water activity at Gale crater on Mars. Nat. Geosci. 2015, 8, 357–361. [Google Scholar] [CrossRef] [Scilit]
  29. Wilks, J.M.; Chen, F.; Clark, B.C.; Schneegurt, M.A. Bacterial growth in saturated and eutectic solutions of magnesium sulphate and potassium chlorate with relevance to Mars and the ocean worlds. Int. J. Astrobiol. 2019, 18, 502–509. [Google Scholar] [CrossRef] [Scilit]
  30. Cockell, C.S.; Catling, D.C.; Davis, W.L.; Snook, K.; Kepner, R.L.; Lee, P.; McKay, C.P. The Ultraviolet Environment of Mars: Biological Implications Past, Present, and Future. Icarus 2000, 146, 343–359. [Google Scholar] [CrossRef] [Scilit]
  31. Hallsworth, J.E.; Koop, T.; Dallas, T.D.; Zorzano, M.-P.; Burkhardt, J.; Golyshina, O.V.; Martín-Torres, J.; Dymond, M.K.; Ball, P.; McKay, C.P. Water activity in Venus’s uninhabitable clouds and other planetary atmospheres. Nat. Astron. 2021, 5, 665–675. [Google Scholar] [CrossRef] [Scilit]
  32. McKay, C.P.; Smith, H.D. Possibilities for methanogenic life in liquid methane on the surface of Titan. Icarus 2005, 178, 274–276. [Google Scholar] [CrossRef] [Scilit]
  33. Lasne, J.; McCoustra, M.R.S.; Rosu-Finsen, A.; Romanias, M.N.; Lefèvre, F. Editorial: Heterogeneous processes on dust and ice surfaces in planetary atmospheres: Mars, Venus, Titan, and perspectives for exoplanets. Front. Astron. Space Sci. 2023, 9, 1106484. [Google Scholar] [CrossRef] [Scilit]
  34. Certini, G.; Karunatillake, S.; Zhao, Y.-Y.S.; Meslin, P.-Y.; Cousin, A.; Hood, D.R. Disambiguating the soils of Mars, Planet. Space Sci. 2020, 186, 104922. [Google Scholar] [CrossRef] [Scilit]
  35. Rafkin, S.C.R. The potential importance of non-local, deep transport on the energetics, momentum, chemistry, and aerosol distributions in the atmospheres of Earth, Mars, and Titan, Planet. Space Sci. 2012, 60, 147–154. [Google Scholar] [CrossRef] [Scilit]
  36. Gómez, F.; Rodríguez-Manfredi, J.A.; Rodríguez, N.; Fernández-Sampedro, M.; Caballero-Castrejón, F.J.; Amils, R. Habitability: Where to look for life? Halophilic habitats: Earth analogs to study Mars habitability. Planet. Space Sci. 2012, 68, 48–55. [Google Scholar] [CrossRef] [Scilit]
  37. Hurowitz, J.A.; Grotzinger, J.P.; Fischer, W.W.; McLennan, S.M.; Milliken, R.E.; Stein, N.; Vasavada, A.R.; Blake, D.F.; Dehouck, E.; Eigenbrode, J.L.; et al. Redox stratification of an ancient lake in Gale crater, Mars. Science 2017, 356, eaah6849. [Google Scholar] [CrossRef] [Scilit]
  38. Seto, M.; Noguchi, K.; Cappellen, P.V. Potential for Aerobic Methanotrophic Metabolism on Mars. Astrobiology 2019, 19, 1187–1195. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. King, G.M. Carbon monoxide as a metabolic energy source for extremely halophilic microbes: Implications for microbial activity in Mars regolith. Proc. Natl. Acad. Sci. USA 2015, 112, 4465–4470. [Google Scholar] [CrossRef] [Scilit]
  40. Davila, A.F.; Schulze-Makuch, D. The Last Possible Outposts for Life on Mars. Astrobiology 2016, 16, 159–168. [Google Scholar] [CrossRef] [Scilit]
  41. Waite, J.H.; Young, D.T.; Cravens, T.E.; Coates, A.J.; Crary, F.J.; Magee, B.; Westlake, J. The Process of Tholin Formation in Titan’s Upper Atmosphere. Science 2007, 316, 870–875. [Google Scholar] [CrossRef] [Scilit]
  42. Maillard, J.; Hupin, S.; Carrasco, N.; Schmitz-Afonso, I.; Gautier, T.; Afonso, C. Structural elucidation of soluble organic matter: Application to Titan’s haze. Icarus 2020, 340, 113627. [Google Scholar] [CrossRef] [Scilit]
  43. Young, A.T. Venus clouds: Structure and composition. Science 1974, 183, 407–409. [Google Scholar] [CrossRef] [Scilit]
  44. Cockell, C.S.; Higgins, P.M.; Johnstone, A.A. Biologically Available Chemical Energy in the Temperate but Uninhabitable Venusian Cloud Layer: What Do We Want to Know? Astrobiology 2021, 21, 1224–1236. [Google Scholar] [CrossRef] [Scilit]
  45. Kimura, J. Icy Worlds: Moons and Dwarf Planets. In Oxford Research Encyclopedia of Planetary Science; Read, P., Ed.; Oxford University Press: Oxford, UK, 2017. [Google Scholar]
  46. Villanueva, G.L.; Hammel, H.B.; Milam, S.N.; Kofman, V.; Faggi, S.; Glein, C.R.; Cartwright, R.; Roth, L.; Hand, K.P.; Paganini, L.; et al. JWST molecular mapping and characterization of Enceladus’ water plume feeding its torus. Nat. Astron. 2023, 7, 1056–1062. [Google Scholar] [CrossRef] [Scilit]
  47. Hand, K.P.; Chyba, C.F.; Carlson, R.W.; Cooper, J.F. Clathrate hydrates of oxidants in the ice shell of Europa. Astrobiology 2006, 6, 463–482. [Google Scholar] [CrossRef] [Scilit]
  48. Grant, W.D. Life at low water activity. Philos. Trans. R. Soc. B Biol. Sci. 2004, 359, 1249–1267. [Google Scholar] [CrossRef] [Scilit]
  49. Stevenson, A.; Cray, J.A.; Williams, J.P.; Santos, R.; Sahay, R.; Neuenkirchen, N.; McClure, C.D.; Grant, I.R.; Houghton, J.D.; Quinn, J.P.; et al. Is there a common water-activity limit for the three domains of life? ISME J. 2015, 9, 1333–1351. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Potts, M. Desiccation tolerance of prokaryotes. Microbiol. Rev. 1994, 58, 755–805. [Google Scholar] [CrossRef]
  51. Pastor, J.M.; Salvador, M.; Argandoña, M.; Bernal, V.; Reina-Bueno, M.; Csonka, L.N.; Iborra, J.L.; Vargas, C.; Nieto, J.J.; Cánovas, M. Ectoines in cell stress protection: Uses and biotechnological production. Biotechnol. Adv. 2010, 28, 782–801. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  52. Czech, L.; Hermann, L.; Stöveken, N.; Richter, A.A.; Höppner, A.; Smits, S.H.J. Role of the Extremolytes Ectoine and Hydroxyectoine as Stress Protectants and Nutrients: Genetics, Phylogenomics, Biochemistry, and Structural Analysis. Genes 2018, 9, 177. [Google Scholar] [CrossRef] [Scilit]
  53. Crowe, J.H.; Carpenter, J.F.; Crowe, L.M. The role of vitrification in anhydrobiosis. Annu. Rev. Physiol. 1998, 60, 73–103. [Google Scholar] [CrossRef] [Scilit]
  54. Marks, R.A.; Ekwealor, J.T.B.; Artur, M.A.S.; Bondi, L.; Boothby, T.C.; Carmo, O.M.S.; Centeno, D.C.; Coe, K.K.; Dace, H.J.W.; Field, S.; et al. Life on the dry side: A roadmap to understanding desiccation tolerance and accelerating translational applications. Nat. Commun. 2025, 16, 3284. [Google Scholar] [CrossRef] [Scilit]
  55. Daly, M.J. A new perspective on radiation resistance based on Deinococcus radiodurans. Nat. Rev. Microbiol. 2009, 7, 237–245. [Google Scholar] [CrossRef] [Scilit]
  56. Setlow, P. Spores of Bacillus subtilis: Their resistance to and killing by radiation, heat and chemicals. J. Appl. Microbiol. 2006, 101, 514–525. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  57. Hassler, D.M.; Zeitlin, C.; Wimmer-Schweingruber, R.F.; Ehresmann, B.; Rafkin, S.; Eigenbrode, J.L.; Brinza, D.E.; Weigle, G.; Böttcher, S.; Böhm, E.; et al. Mars’ Surface Radiation Environment Measured with the Mars Science Laboratory’s Curiosity Rover. Science 2014, 343, 1244797. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  58. Setlow, R.B. Cyclobutane-Type Pyrimidine Dimers in Polynucleotides. Science 1966, 153, 379–386. [Google Scholar] [CrossRef] [Scilit]
  59. Billi, D.; Viaggiu, E.; Cockell, C.S.; Rabbow, E.; Horneck, G.; Onofri, S. Damage escape and repair in dried Chroococcidiopsis spp. from hot and cold deserts exposed to simulated space and martian conditions. Astrobiology 2011, 11, 65–73. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  60. Flemming, H.-C.; Wingender, J. The biofilm matrix. Nat. Rev. Microbiol. 2010, 8, 623–633. [Google Scholar] [CrossRef] [Scilit]
  61. Hecht, M.H.; Kounaves, S.P.; Quinn, R.C.; West, S.J.; Young, S.M.M.; Ming, D.W. Detection of Perchlorate and the Soluble Chemistry of Martian Soil at the Phoenix Lander Site. Science 2009, 325, 64–67. [Google Scholar] [CrossRef] [Scilit]
  62. Coates, J.D.; Achenbach, L.A. Microbial perchlorate reduction: Rocket-fuelled metabolism. Nat. Rev. Microbiol. 2004, 2, 569–580. [Google Scholar] [CrossRef] [Scilit]
  63. Johnson, D.B.; Hallberg, K.B. The microbiology of acidic mine waters. Res. Microbiol. 2003, 154, 466–473. [Google Scholar] [CrossRef] [Scilit]
  64. D’Amico, S.; Collins, T.; Marx, J.; Feller, G.; Gerday, C.; Gerday, C. Psychrophilic microorganisms: Challenges for life. EMBO Rep. 2006, 7, 385–389. [Google Scholar] [CrossRef] [Scilit]
  65. Cable, M.L.; Hörst, S.M.; Hodyss, R.; Beauchamp, P.M.; Smith, M.A.; Willis, P.A. Titan Tholins: Simulating Titan Organic Chemistry in the Cassini-Huygens Era. Chem. Rev. 2012, 112, 1882–1909. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  66. Bosak, T.; Moore, K.R.; Gong, J.; Grotzinger, J.P. Searching for biosignatures in sedimentary rocks from early Earth and Mars. Nat. Rev. Earth Environ. 2021, 2, 490–506. [Google Scholar] [CrossRef] [Scilit]
  67. McMahon, S.; Ivarsson, M.; Wacey, D.; Saunders, M.; Belivanova, V.; Muirhead, D. Dubiofossils from a Mars-analogue subsurface palaeoenvironment: The limits of biogenicity criteria. Geobiology 2021, 19, 473–488. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  68. Rothschild, L.J.; Mancinelli, R.L. Life in extreme environments. Nature 2001, 409, 1092–1101. [Google Scholar] [CrossRef] [Scilit]
  69. Meola, M.; Lazzaro, A.; Zeyer, J. Bacterial Composition and Survival on Sahara Dust Particles Transported to the European Alps. Front. Microbiol. 2015, 6, 1454. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  70. De Micco, V.; Amitrano, C.; Mastroleo, F.; Aronne, G.; Battistelli, A.; Carnero-Diaz, E.; De Pascale, S.; Detrell, G.; Dussap, C.G.; Ganigué, R.; et al. Plant and microbial science and technology as cornerstones to Bioregenerative Life Support Systems in space. npj Microgravity 2023, 9, 69. [Google Scholar] [CrossRef] [Scilit]
  71. Anabtawi, H.M.; Ikhlaq, A.; Kumar, S.; Rafique, S.; Hassan, A.A. Addressing Challenges for Eco-Friendly and Sustainable Wastewater Treatment Solutions Using Extremophile Microorganisms. Sustainability 2025, 17, 2339. [Google Scholar] [CrossRef] [Scilit]
  72. Esposito, M.; Tonietti, L.; Santomartino, R.; Giovannelli, D.; Chianese, E.; Rotundi, A. Integrating resource utilization and bioregenerative life support systems for sustainable space exploration. Front. Microbiol. 2026, 17, 1837116. [Google Scholar] [CrossRef] [Scilit]
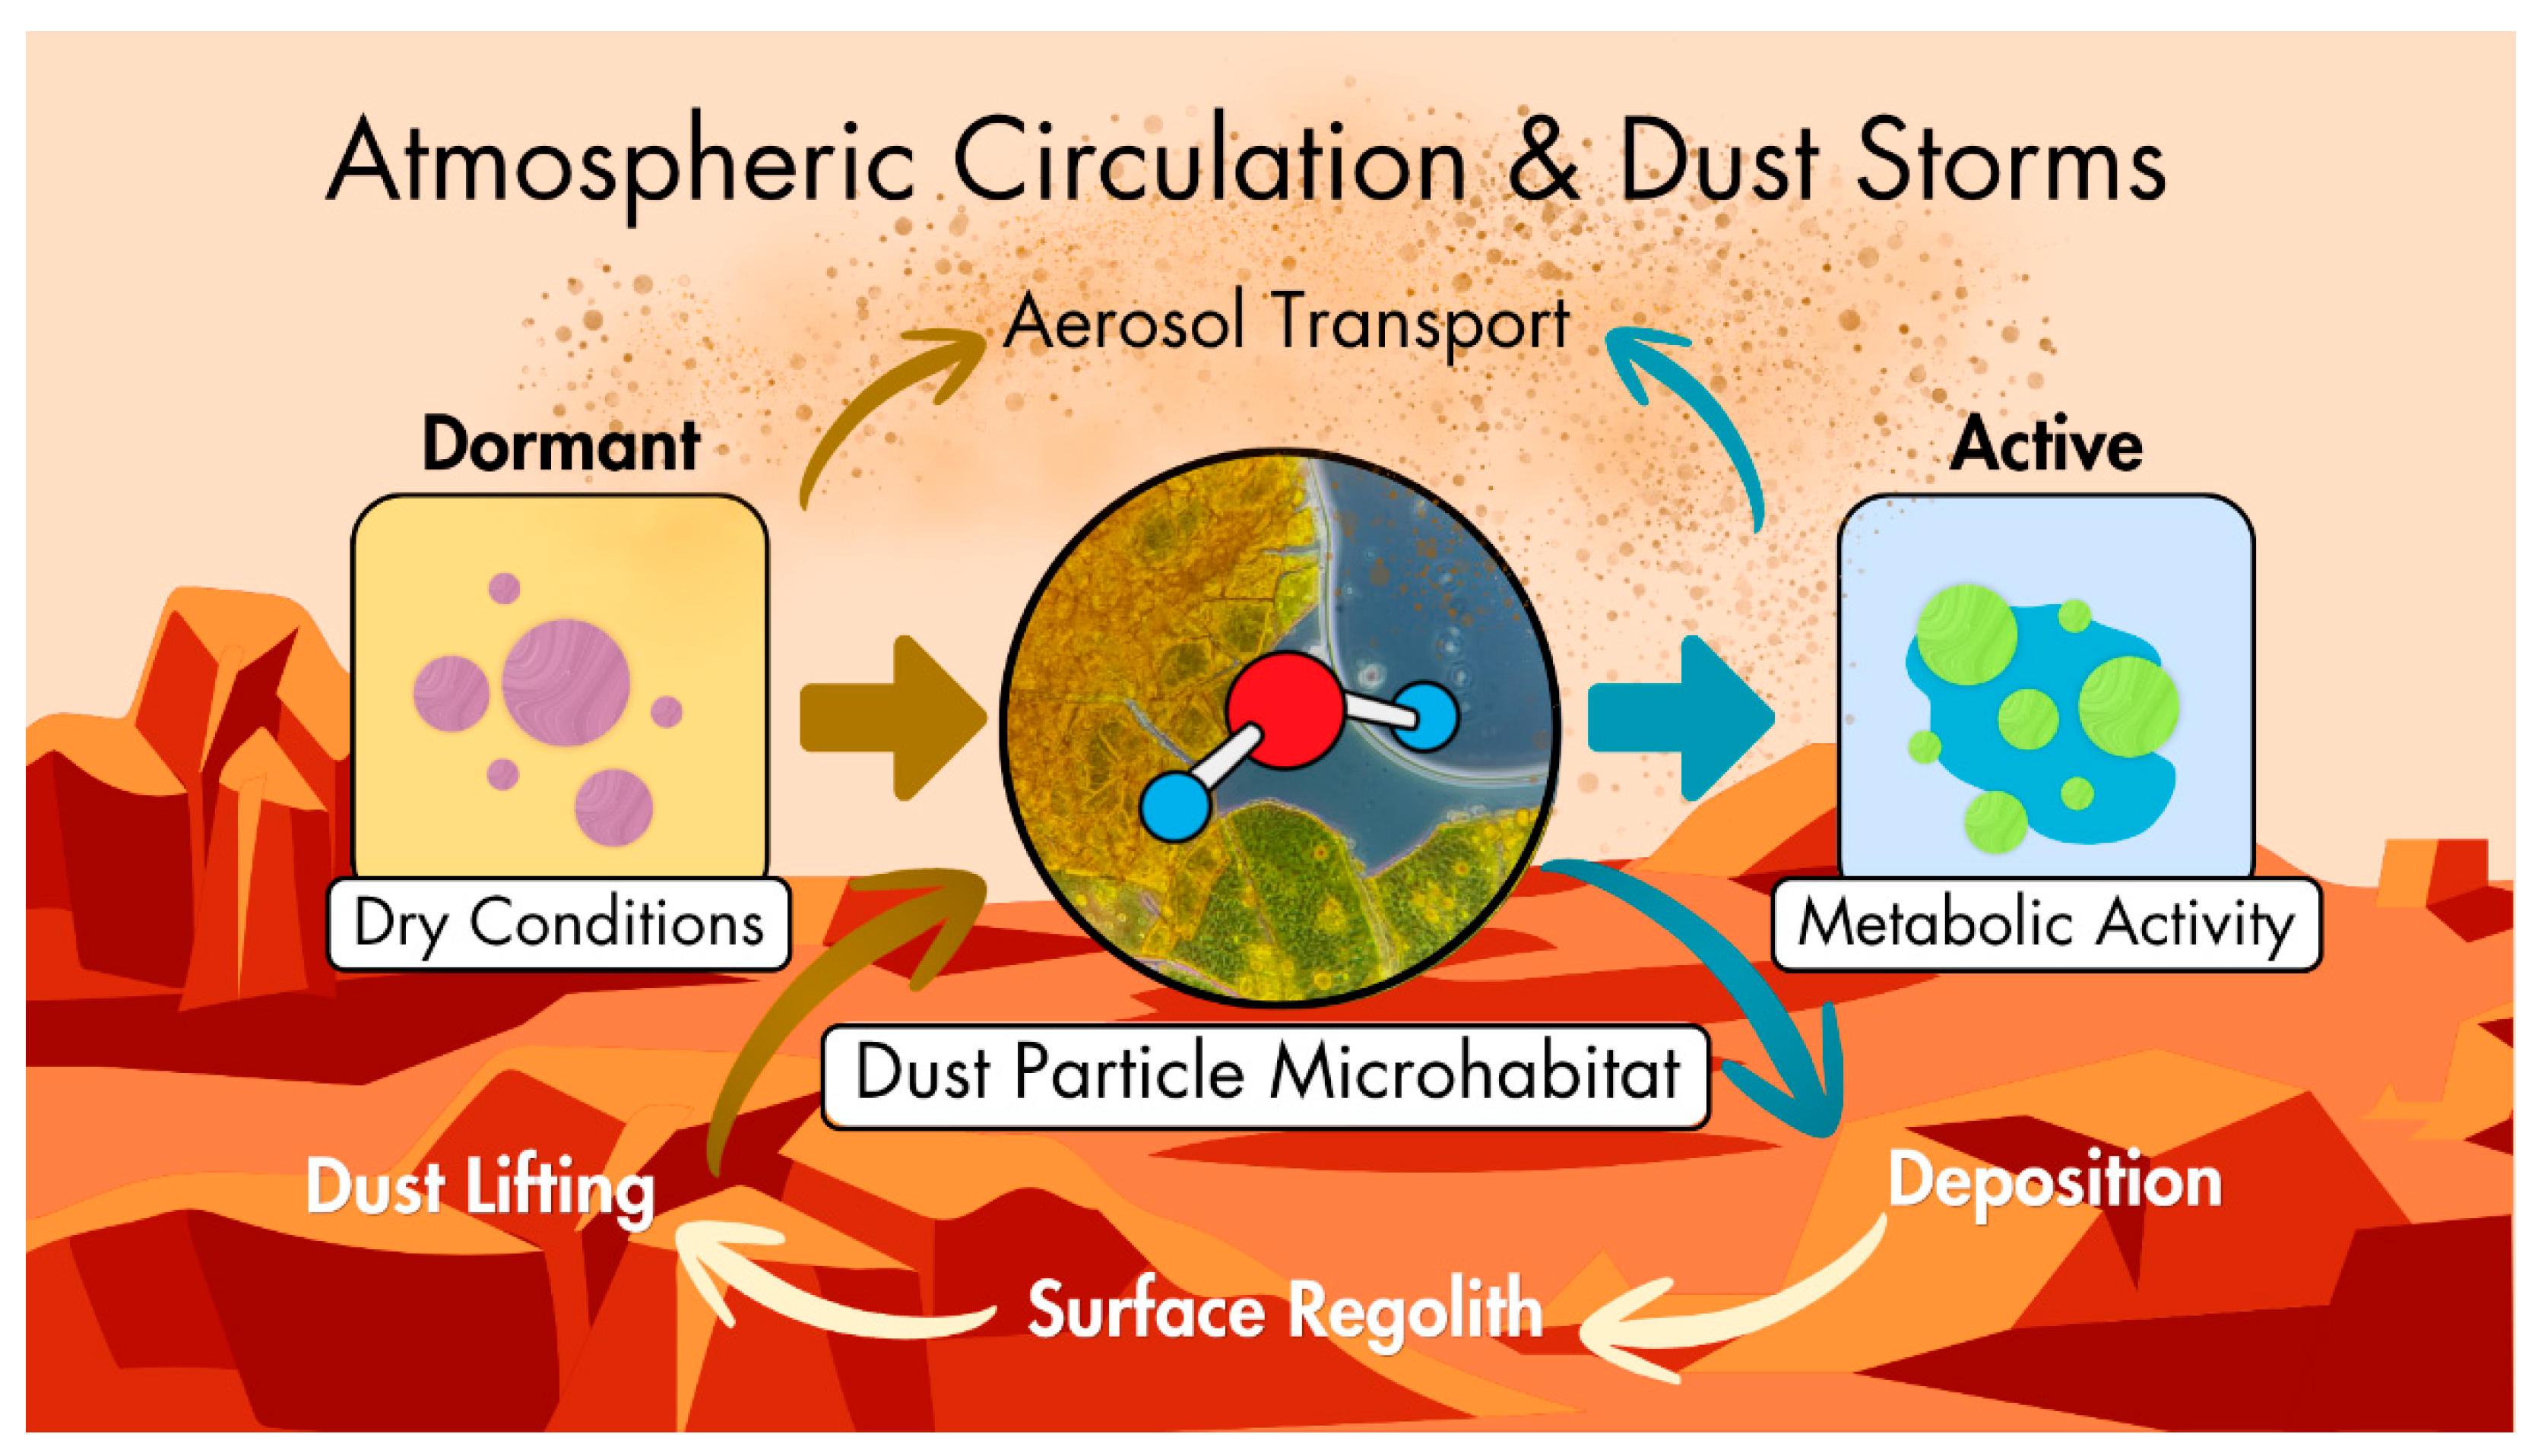
Figure 1. Conceptual model of a planetary aerobiome. Atmospheric circulation lifts refractory dust particles from the surface, transporting them through the atmosphere before deposition. Refractory dust particles act as mobile particle-associated microenvironments that can host microorganisms in dormant states under dry conditions and enable episodic metabolic activity during transient hydration. This cycle of lifting, transport, activation, and settling creates a distributed, particle-associated microbial system.
Applmicrobiol 06 00066 g001
Table 1. Summary of discussed planetary bodies where atmospheric particles or surface-derived grains may act as microhabitats for microbial survival and dispersal. For each environment, the dominant particle environment, potential microhabitat, and possible biological processes are indicated, highlighting the broad applicability of the planetary aerobiome concept across the Solar System.
Planetary BodyParticle EnvironmentMicrohabitatBiological ProcessesRelevance to Aerobiome Concept
MarsRefractory dustMineral grainsDormancy, lithotrophyGlobal dispersal system
TitanAerosol particlesOrganic-rich aerosol particlesMethanogenesis/methanotrophyAtmospheric ecosystem
VenusAcid aerosol dropletsH2SO4-rich dropletsAcidic resistance/adapted molecular structures and metabolismsAcid aerosol-associated persistence system
Icy MoonsIce grains/plume particlesIce grainsTrasport of organicsOcean-surface coupling
Table 2. Overview of biosignature types that may be preserved or transported within atmospheric particles, including refractory dust and aerosol particles. Morphological, molecular, isotopic, and mineral–organic indicators are listed together with analytical approaches that could be employed in future life-detection missions.
Biosignature TypeIndicatorDetection MethodRelevance for Aerobiomes
MorphologicalCell-like
structures
MicroscopyDirect evidence of particle-
associated life
MolecularOrganics (lipids, pigments, etc.)SpectroscopyPreserved biomolecules in dust
IsotopicFractionationMass
spectrometry
Metabolic signatures
Mineral–organicCoatings,
interfaces
RAMAN/SEMBio-mineral interaction
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.



