Article

New Insights into Mousterian Faunal Assemblages from Uluzzo C (Apulia, Southern Italy)

by
Angelica Fiorillo
1,*,†,
Silvia Irina Monterrosa Preziosi
1,†,
Sara Silvestrini
1,
Lisa Brotons
1,2,
Gruppo Speleologico Neretino
3,
Enza Elena Spinapolice
4,
Omry Barzilai
5,
Francesco Berna
6,7,
Adriana Moroni
6,8,9,
Matteo Romandini
1,
Gabriele Terlato
1 and
Stefano Benazzi
1
1
Department of Cultural Heritage, University of Bologna, Via degli Ariani 1, 48121 Ravenna, Italy
2
Department of Chemistry “Giacomo Ciamician”, University of Bologna, Via Guaccimanni 42, 48121 Ravenna, Italy
3
Piazza Cesare Battisti, 73048 Nardò, Italy
4
Department of Ancient World Studies, Sapienza University of Rome, Piazzale Aldo Moro 5, 00185 Rome, Italy
5
Material Culture PaleoLab, The Leon Recanati Institute for Maritime Studies, School of Archaeology and Maritime Cultures, University of Haifa, Mt. Carmel, Haifa 3103301, Israel
6
Department of Physical Science, Earth and Environment, University of Siena 1240, Strada Laterina 8, 53100 Siena, Italy
7
Department of Archaeology, Simon Fraser University, 8888 University Drive, Burnaby, BC V5A 1S6, Canada
8
Centro Studi Sul Quaternario ODV, Via Nuova dell’Ammazzatoio, 7, Sansepolcro, 52037 Arezzo, Italy
9
Istituto Italiano di Paleontologia Umana, Piazza Ruggero Bonghi, 2, 03012 Anagni, Italy
*
Author to whom correspondence should be addressed.
These authors contributed equally to this work.
Quaternary 2026, 9(3), 37; https://doi.org/10.3390/quat9030037
Submission received: 1 April 2026 / Revised: 2 May 2026 / Accepted: 4 May 2026 / Published: 8 May 2026

Abstract

Grotta-Riparo di Uluzzo C (Uluzzo Bay, Apulia, southern Italy) preserves a long and complex stratigraphic sequence spanning from the Middle Palaeolithic to the Bronze Age, offering a valuable context for investigating depositional dynamics and human–environment interactions during the Late Pleistocene. Although recent multidisciplinary research has substantially advanced knowledge of the Uluzzian occupations, the Mousterian faunal record of the site has remained largely unexplored from zooarchaeological and taphonomic perspectives. This study examines the faunal assemblages from the Mousterian layers (E, F, and G), integrating material from historical excavations with those recovered during recent fieldwork. Zooarchaeological, taphonomic, and Zooarchaeology by Mass Spectrometry (ZooMS) analyses are combined to reconstruct local environmental conditions, evaluate the relative contribution of human and non-human agents to bone accumulation, and assess patterns of site use and deposit formation. The faunal spectrum indicates an ecologically heterogeneous landscape, consistent with a Mediterranean refugial setting during the Late Pleistocene. Taphonomic evidence points to complex and cumulative formation processes resulting from repeated, short-term human occupations interspersed with carnivore activity and natural depositional processes. The Mousterian deposits are therefore best interpreted as brief palimpsests rather than the result of continuous or intensive occupation. Placed within a regional framework, the Uluzzo C assemblages contribute to broader discussions on site formation processes and environmental variability in southern Italy and provide an important comparative baseline for the Middle to Upper Palaeolithic period.

1. Introduction

Faunal assemblages recovered from caves and rock shelters represent one of the primary datasets for investigating human–environment interactions and site formation processes during the Late Pleistocene. However, their interpretative potential critically depends on the recognition and disentanglement of multiple accumulating agents and post-depositional processes that often operate within the same stratigraphic contexts. In caves and rock shelters, Mousterian occupations commonly form stratigraphic successions resulting from recurrent and often alternating use by human groups and carnivores over more or less extended periods of time, frequently characterised by short-term and discontinuous occupations ([1,2,3,4,5,6], among others). In these contexts, the cumulative nature of the archaeological record intersects with issues of temporal resolution and cultural attribution, as well as with questions related to the Neanderthal–Sapiens relationships and variability in occupation intensity [7,8].
Within this interpretative framework, reconstructing human subsistence strategies is essential. Archaeological consensus has long held that Neanderthals relied predominantly on ungulates and other large game across much of Eurasia ([9,10,11,12,13,14,15,16,17,18,19,20,21,22,23], among others). However, an expanding body of evidence indicates that Late Pleistocene human groups also exploited plant resources and a wide range of small and medium-sized prey, including tortoises, birds, small game and marine resources, including molluscs [1,24,25,26,27,28,29,30,31,32,33,34,35,36,37,38,39,40], challenging long-standing assumptions about regional dietary variability and suggesting that Neanderthal diets were broader than previously recognised. At the scale of the Mediterranean Basin, recent case studies further clarify this variability, documenting small-game use and freshwater/coastal fishing at several Late Pleistocene sites [39,41,42,43,44].
Southern Italy, and Apulia in particular, offers an exceptional setting for investigating Neanderthal lifestyles and adaptations to climate and environment. The abundance of archaeological sites with stratified Mousterian levels indicates a continuous Neanderthal presence in the region during the Late Pleistocene, spanning from MIS 5 to mid MIS 3 [45,46,47], until their abandonment of those territories just before or during the arrival of modern humans [48,49,50]. Apulia may have served as a refugium when thermophilous and temperate species migrated southwards [46,48], thereby ensuring the persistence, conservation and survival of biodiversity, including plant species, animal species and human populations [49,50]. Numerous Mousterian sites in Apulia document repeated human occupation within ecologically heterogeneous landscapes [51,52], yet zooarchaeological studies highlight substantial variability in the relative contribution of anthropogenic and non-anthropogenic agents to faunal assemblages across sites and stratigraphic units [46,53,54,55].
Within this regional framework, Grotta-Riparo di Uluzzo C (hereinafter Uluzzo C) represents a key site for investigating Middle Palaeolithic dynamics within a long and well-stratified sequence spanning from the Mousterian to the Bronze Age. Excavations carried out in the 1960s by Borzatti [56,57,58] established the stratigraphic framework and documented the importance of the Mousterian deposits (layers E, F, and G), although the associated faunal assemblages were never subjected to systematic zooarchaeological and taphonomic analysis. For decades, the presumed loss of the assemblage prevented any reassessment using modern analytical approaches. The recent relocation of the faunal collection from the 1960s excavations now makes it possible to address this gap and to apply integrated zooarchaeological, taphonomic, and biomolecular analyses, including Zooarchaeology by Mass Spectrometry (ZooMS), allowing for the taxonomic identifications where morphological criteria alone are insufficient. Since 2016, renewed multidisciplinary research at Uluzzo C has significantly refined the stratigraphic, chronological, and geoarchaeological framework of the site through new excavations, absolute dating, sedimentological and micromorphological analyses, as well as detailed studies of the lithic industries, faunal remains and pollen [59,60,61,62,63,64,65].
This paper presents the first comprehensive zooarchaeological, taphonomic, and ZooMS-based study of the faunal assemblages from the Mousterian layers (E, F, and G) at Uluzzo C, bridging materials from both historical and recent excavations. Our study aims to reconstruct local palaeoenvironmental conditions, identify the agents responsible for bone accumulation and modification, and assess patterns of hominin site occupation. The results are discussed within a regional and diachronic framework, enabling direct comparison with the overlying Uluzzian phases at Uluzzo C and with other Mousterian assemblages across southern Italy, and contributing to a broader understanding of Neanderthal behavioural and ecological variability in the region.

2. The Archaeological Setting

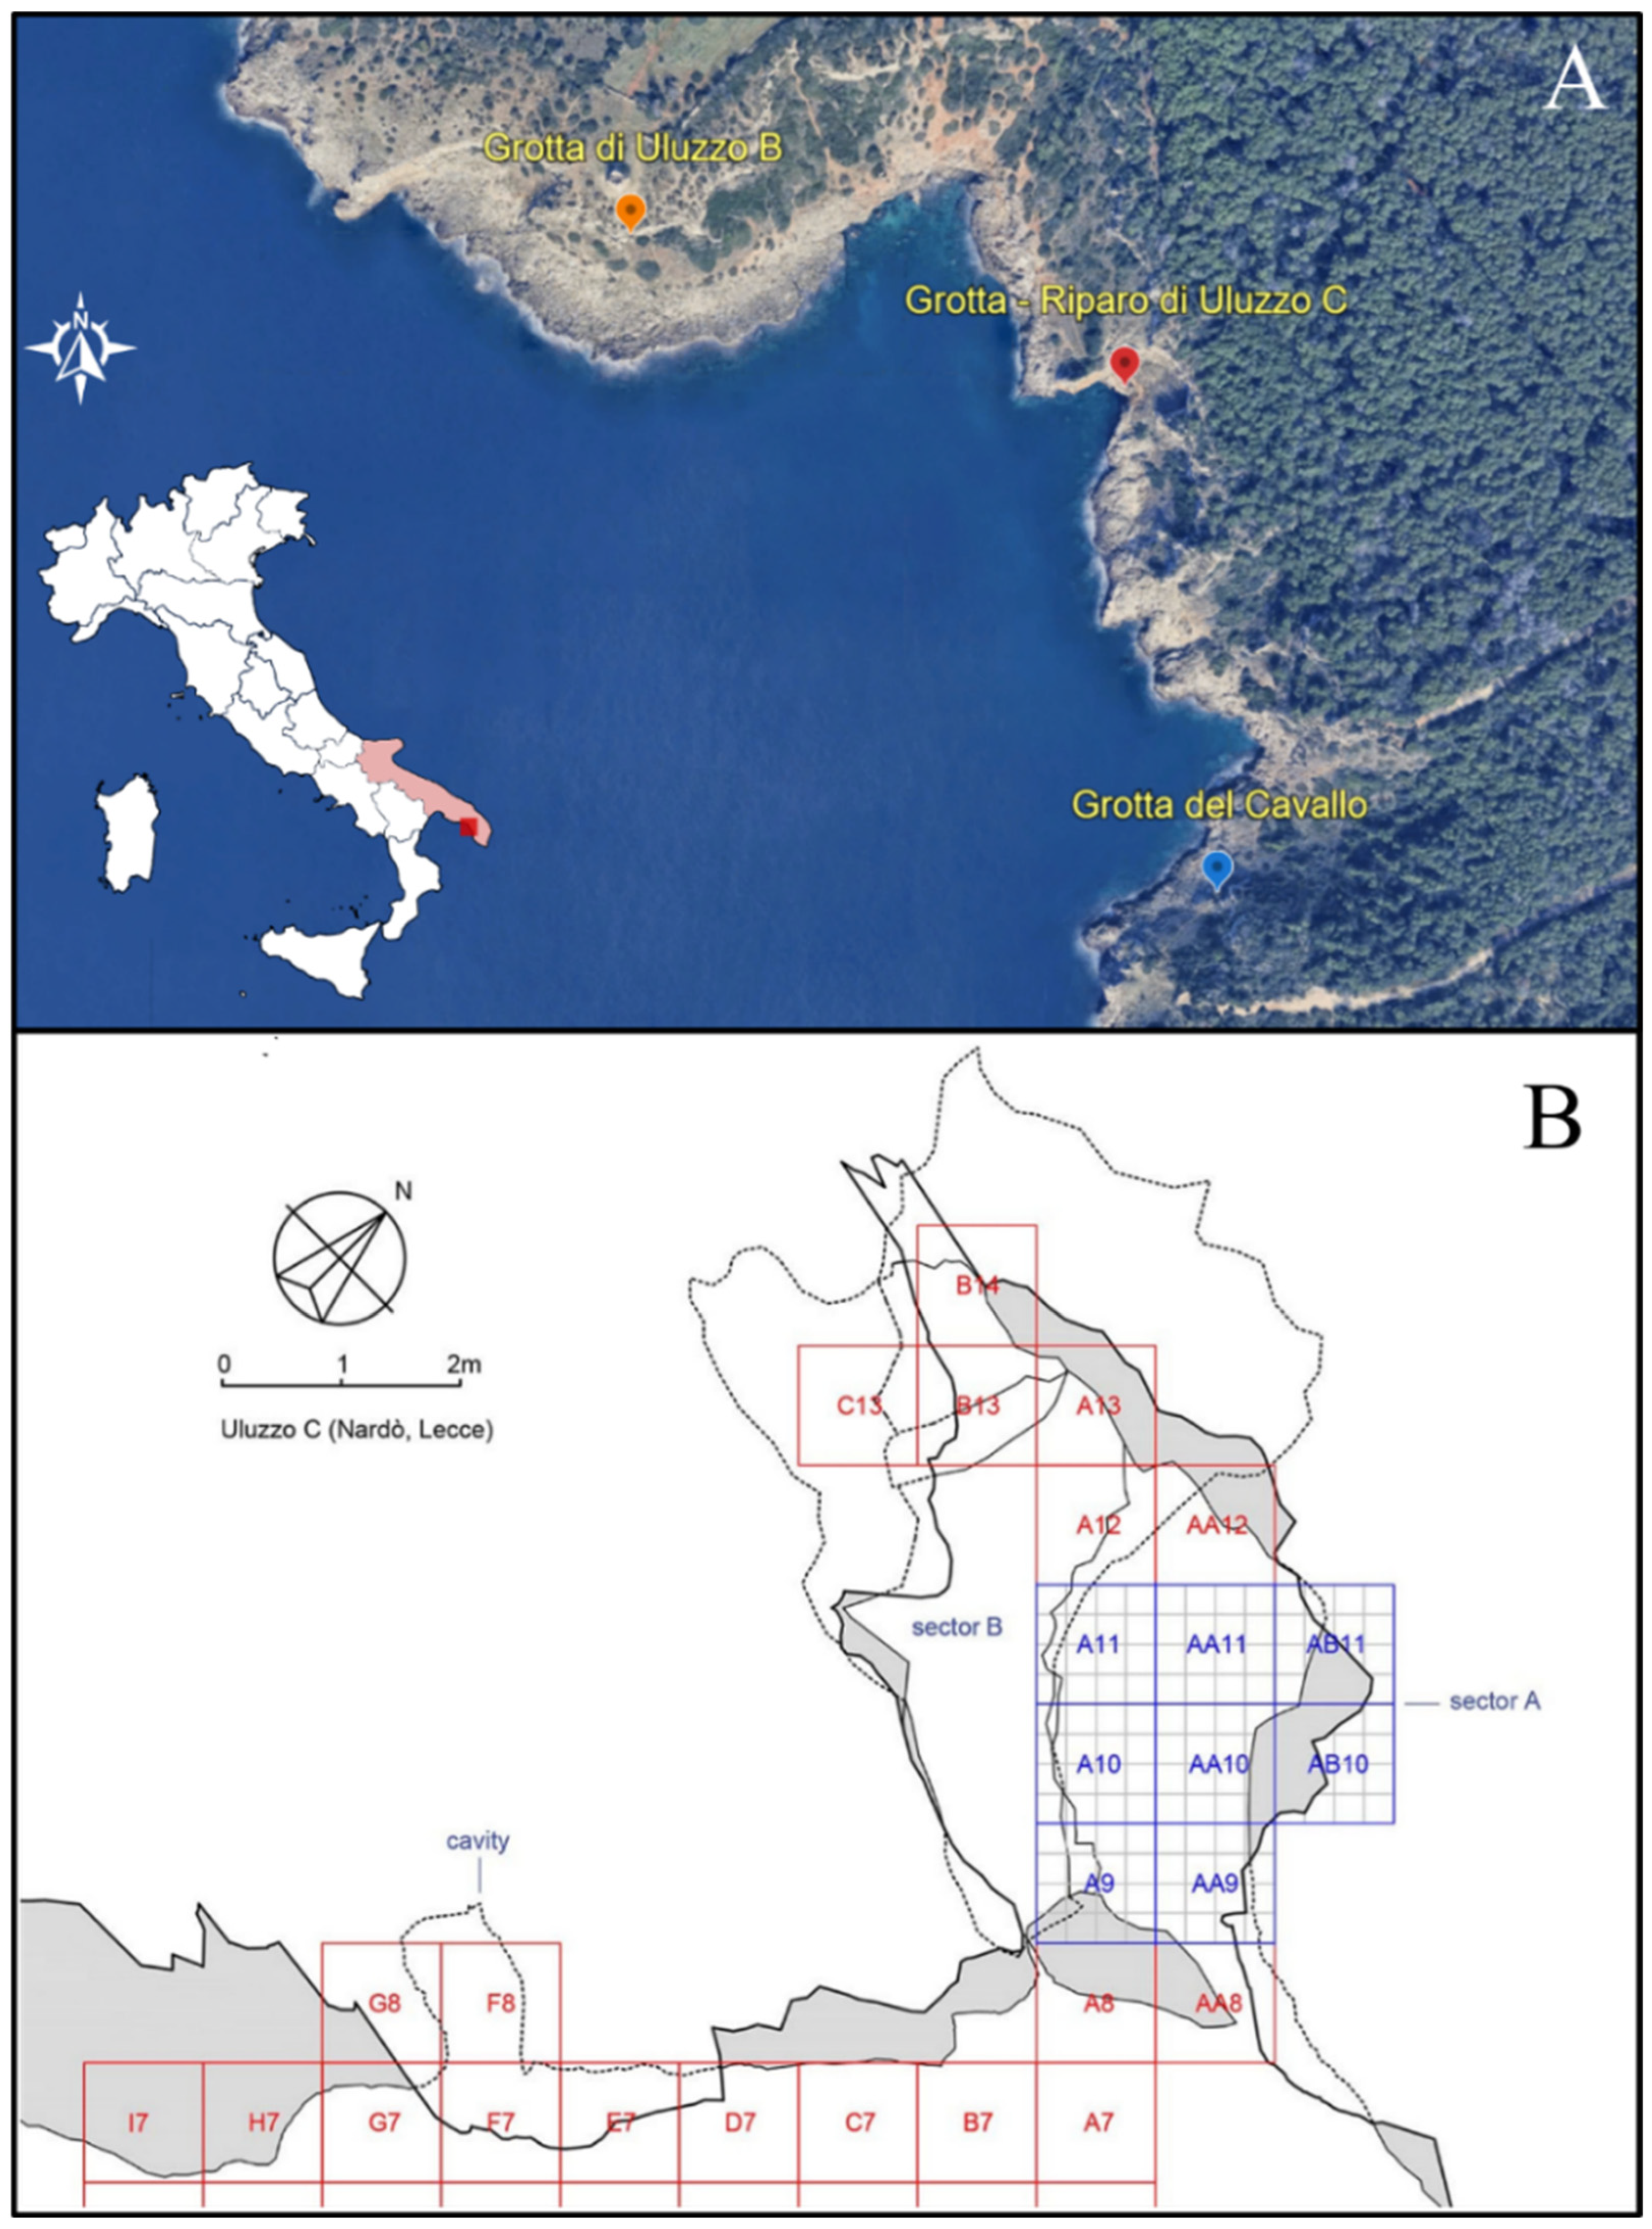
Uluzzo C is located in Nardò, province of Lecce in southern Italy, along the western Apulian coastline overlooking the Ionian Sea (40°9′27.84″ N, 17°57′35.34″ E). It is situated within the Parco Naturale di Porto Selvaggio, in the centre of Uluzzo Bay, with the nearby Grotta del Cavallo (Uluzzo A) and Grotta di Uluzzo B located less than 300 m away (Figure 1A). The current configuration of Uluzzo C comprises a narrow central hall alongside an external sedimentary deposit that rests against the rock face and slopes downward toward the sea. These elements constitute the preserved portions of what was originally a more spacious cave and shelter system that experienced vault failure [56,57,58].
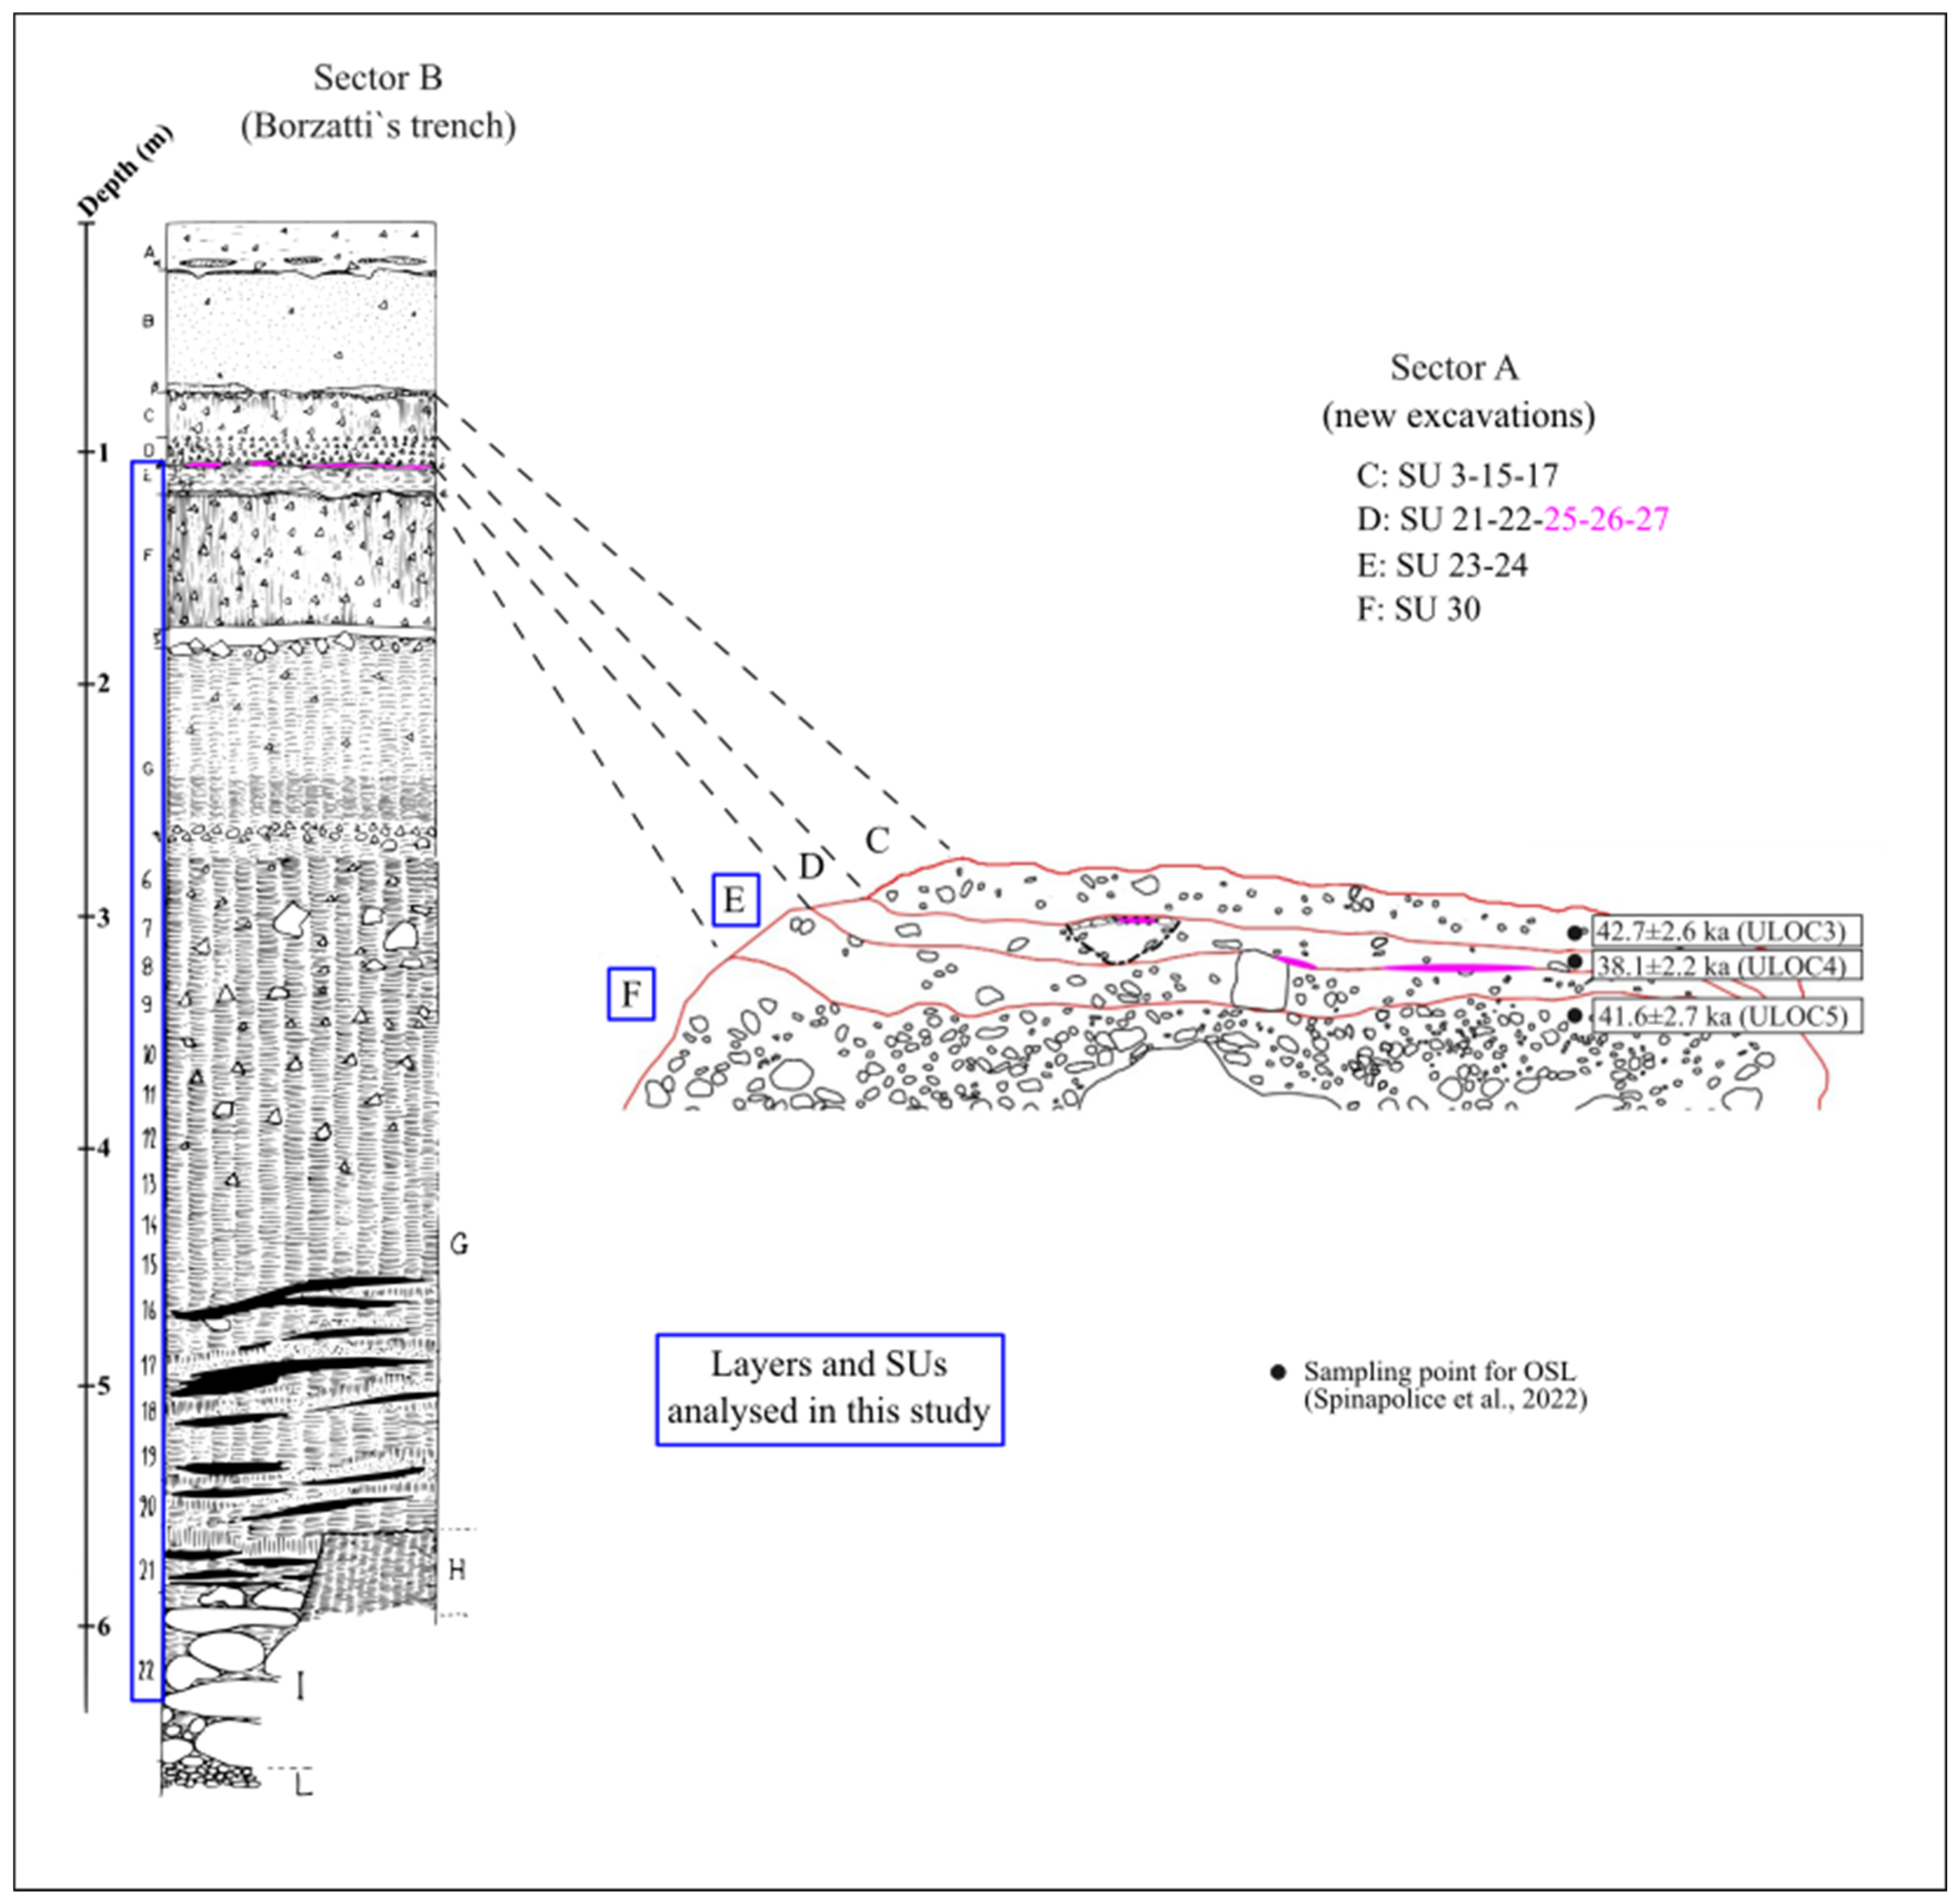
The site was first identified in 1960 when Carlo Cosma and the Gruppo Speleologico Salentino conducted a survey of caves in Uluzzo Bay. During these explorations, lithic artefacts, abundant faunal remains, and human teeth, recently morphometrically attributed to Neanderthals [61], were recovered [66]. Systematic stratigraphic excavations were conducted at Uluzzo C between 1963 and 1968 under the direction of Edoardo Borzatti von Löwerstern, carried out by the Italian Institute of Prehistory and Protohistory (IIPP) of Florence in collaboration with the Provincial Administration of Lecce and the “S. Castromediano” Archaeological Museum [56,57,58]. During the initial phase of fieldwork (1963–1966), a 2.6 × 1.5 m trench was opened in the central portion of the deposit, extending to a depth of 2.5 m (Sector B, Figure 1B) and revealing a continental sequence spanning from the Mousterian to the Bronze Age. This trench was later enlarged to a depth of about 6 m, until a marine deposit was identified by Borzatti von Löwerstern as a Tyrrhenian beach. The uppermost units, associated with Bronze Age occupation, had been heavily disturbed by looting, resulting in the loss of most deposits [65]. Two further campaigns were undertaken in 1967 and 1968, extending the trench one meter seaward. This area yielded markedly fewer lithic and faunal materials, despite sedimentological continuity with the interior deposits [56,57,58]. The stratified deposit excavated in the 1960s comprised a sequence approximately 6.40 m thick, divided into ten layers (Figure 2, Table 1). Several units were culturally attributed to Romanellian (layer A) and Uluzzian occupations (layers C and D) as well as an extensive Mousterian sequence (layers E, F, G and H). Intervening sterile sediments (layers B, I, and L) and thin volcanic ash lenses designated by Greek letters (β and γ) completed the sequence [56,57,58].
The new excavations, started in 2016, defined three sectors: A, B, and C (Figure 1B). Sectors A and B lie within the rock shelter, corresponding, respectively, to the present-day surface of the deposit and to the base of Borzatti’s original trench. Sector C, a test trench on the terrace outside the shelter, yielded only reworked sediments, capped by cemented breccia [59]. The first phase of renewed fieldwork (2016–2019) focused on the Uluzzian deposits in Sector A, corresponding to SUs 3, 15 and 17 (Borzatti’s layer C) and SUs 21, 22, 23 and 25 (Borzatti’s layer D). These layers were divided into three distinct phases [62,63,64,65]. The second phase (2022–ongoing) targeted the Middle Palaeolithic sequence, including SUs 23 and 24 (Borzatti’s layer E) and SU 30 (Borzatti’s layer F). The Middle Palaeolithic sequence examined in this study exhibits considerable variation in sedimentary properties and archaeological content, while the analysis of the macrofaunal assemblages focuses on layers E, F, and G from Borzatti’s excavation, together with SUs 23, 24, and 30 (Table 1).
Samples for sedimentological analysis and OSL dating (Table 1) were collected from the entire sequence accessible in sector A (Borzatti’s layers B, C–L) [65]. OSL ages were obtained for the Uluzzian units C (42.7 ± 2.6 ka) and D (38.1 ± 2.2 ka) and for the Mousterian units F (41.6 ± 2.7 ka) [65]. The date of 46 ± 4 ka in the uppermost part of G is, for now, considered too recent if compared with the characteristics of the lithic industry and requires further validation [60]. The lower Mousterian levels (spits 21–6 of unit G) are not supported by direct chronologic data and their age is inferred through correlation with Grotta del Cavallo, where U/Th dating of the base of layer M (overlying deposits comparable to layers I and L at Uluzzo C) yielded ages of c. 116 ka [67], indicating a post-Tyrrhenian chronology for the entire Mousterian sequence at both sites ([61], but for a different view see [68]). A key chronostratigraphic marker is the recent identification at Uluzzo C of the PGT/Y-6 tephra layer (SU 27), situated between units D and E. This tephra derives from the Pantelleria eruption, dated to ~45.0–44.9 ka [60]. The same tephra at Grotta del Cavallo marks the end of the Mousterian [69], providing a terminus ante quem for both the sequences. Collectively, these data constrain the Mousterian occupation at Uluzzo C between the post-Tyrrhenian phase (MIS 5) and c. 45 ka (mid MIS 3).
Figure 1. (A) Location of Uluzzo C in the Bay of Uluzzo (Apulia, southern Italy) from Google Earth, with the indication of the nearby Grotta del Cavallo and Grotta di Uluzzo B; (B) Map of the excavation areas ([68], modified).
Quaternary 09 00037 g001
Figure 2. Stratigraphic sequence of Uluzzo C: Sector B (Borzatti’s trench) ([59,60], modified) and Sector A ([63], modified).
Quaternary 09 00037 g002
Table 1. Schematic archaeological sequence ([59,61,63,68,70,71,72], modified).
Borzatti’s LayersNew Excavation (SUs)Depth (cm)Volcanic LayerSedimentOSL Dates (From Sector A)Cultural Attribution
A 0–17αReworked topsoil with blue-coloured volcanic pumiceous sand lenticels (α). Romanellian
B 17–62βVolcanic pumiceous sand mixed with red detrital quartz sand. At the base a thin layer of silvery-grey pumiceous sand (β).ULOC 2= 22± 2 kaSterile
C3, 15, 1762–80 Strongly cemented red sediment with debris.ULOC 3= 42.7 ± 2.6 kaUluzzian
D21, 22, 26 cs (combustion structure)80–90γ (25, 26, 27)Red sandy sediment with fine debris. At the base lenses of greenish pumice sand (γ = SUs 25 and 27). At the top and within the body of the structure (26cs), a lens of pumice and sand mixed with stones fine sediment, yellowish to olive-green in colour and bright in the light, was identified and recorded as SU26 in recent excavations, 2015–2022. SU 27 at the bottom of the deposit is a Tephra layer (PGT/Y-6) originated during the Pantelleria eruption, dated to ca. 45.0-44.9 ka.ULOC 4= 38.1 ± 2.2 kaUluzzian
E23, 2490–100 Cemented red sandy-silty sediment with few debris. Above a thin violaceous clay layer (δ). Mousterian
F30100–150 Strongly cemented red sediment with debris capped by a thin sandy-clayey yellowish layer (ε). Between G and F there is a 15-20 cm gap (ζ) formed by a hollow zone.ULOC 5= 41.6±2.7 kaMousterian
G 165–250 Dark brown loose sandy-clayey sediment with few debris sealed by a horizon rich in large and small stones, slightly cemented. Unit G was divided in 22 spits (each spit is 10-15 cm thick) by Borzatti. Between spits 4 and 5 there is a layer (η) made of often broken and corroded stones and pebbles generally covered with thick patinas of manganese and iron oxides.ULOC 1= 46 ± 4.0 kaMousterian
H Strongly cemented red ochraceous clayey sandy sediment, which lies on a dark, loose, fine sand layer. In lateral contact with spit 21 of layer G, was interpreted as a possible remnant of an older, partially eroded deposit. Mousterian
I A series of large calcareous rock blocks up to 1 m long exhibiting signs of bioerosion (lithodomes).
L Conglomerate of much smaller, more or less rounded blocks, contained in a coarse white predominantly calcareous sand tenaciously cemented and travertinised, with limestone fragments and fossils of marine shells. The marine event represented by layers I and L was attributed by Borzatti to MIS5e, providing a terminus post quem for human occupation, as observed at other Mousterian sites in the region.

3. Materials and Methods

This study examines macrofaunal remains of the Mousterian sequence of Uluzzo C, combining material from two excavation campaigns: 1577 remains from the historical excavations by Borzatti in the 1960s (layers E, F, and G), stored at Museo di Storia Naturale di Firenze, and 1233 remains from the recent investigations initiated in 2016 (stratigraphic units 23, 24, and 30). A total of 2810 faunal remains from the Mousterian layers were analysed using an integrated zooarchaeological and taphonomic approach, complemented by targeted ZooMS (Zooarchaeology by Mass Spectrometry) analysis. The study included all bone fragments, from larger pieces (>20 mm) to identifiable and indeterminate smaller fragments (<20 mm).

3.1. Taxonomic and Anatomical Analysis

Taxonomic and skeletal identifications were carried out in the Bones Lab (Laboratory of Osteoarchaeology and Palaeoanthropology) at the Department of Cultural Heritage of the University of Bologna (Ravenna, Italy), using both the reference collection, osteological atlases [72,73,74,75] and online resources, including 3D model repositories and photographic databases (e.g., Sketchfab.com; boneid.net; vertebres3d.fr; boneidentification.com). Faunal remains were categorised into determinate specimens, identified both taxonomically and anatomically, and indeterminate specimens, for which only anatomical identification, or no identification, was possible. Taxonomically unidentifiable specimens were grouped according to their body size into five mammals categories: size 1: smaller than a rabbit; size 2, small mammals weighing < 20 kg (Lagomorphs, Rodents and small carnivores); size 3, medium mammals between 20 and 100 kg (e.g., Capreolus capreolus, Canis lupus); size 4, medium/large mammals between 100 and 300 kg (e.g., Cervus elaphus, Dama dama, Crocuta spelaea); and size 5, large mammals of >300 kg (e.g., Bos/Bison). When species determination was indeterminate, elements were reported to their family (e.g., Cervidae, Caprinae), genus (e.g., Bos/Bison) or class (e.g., Aves) level.
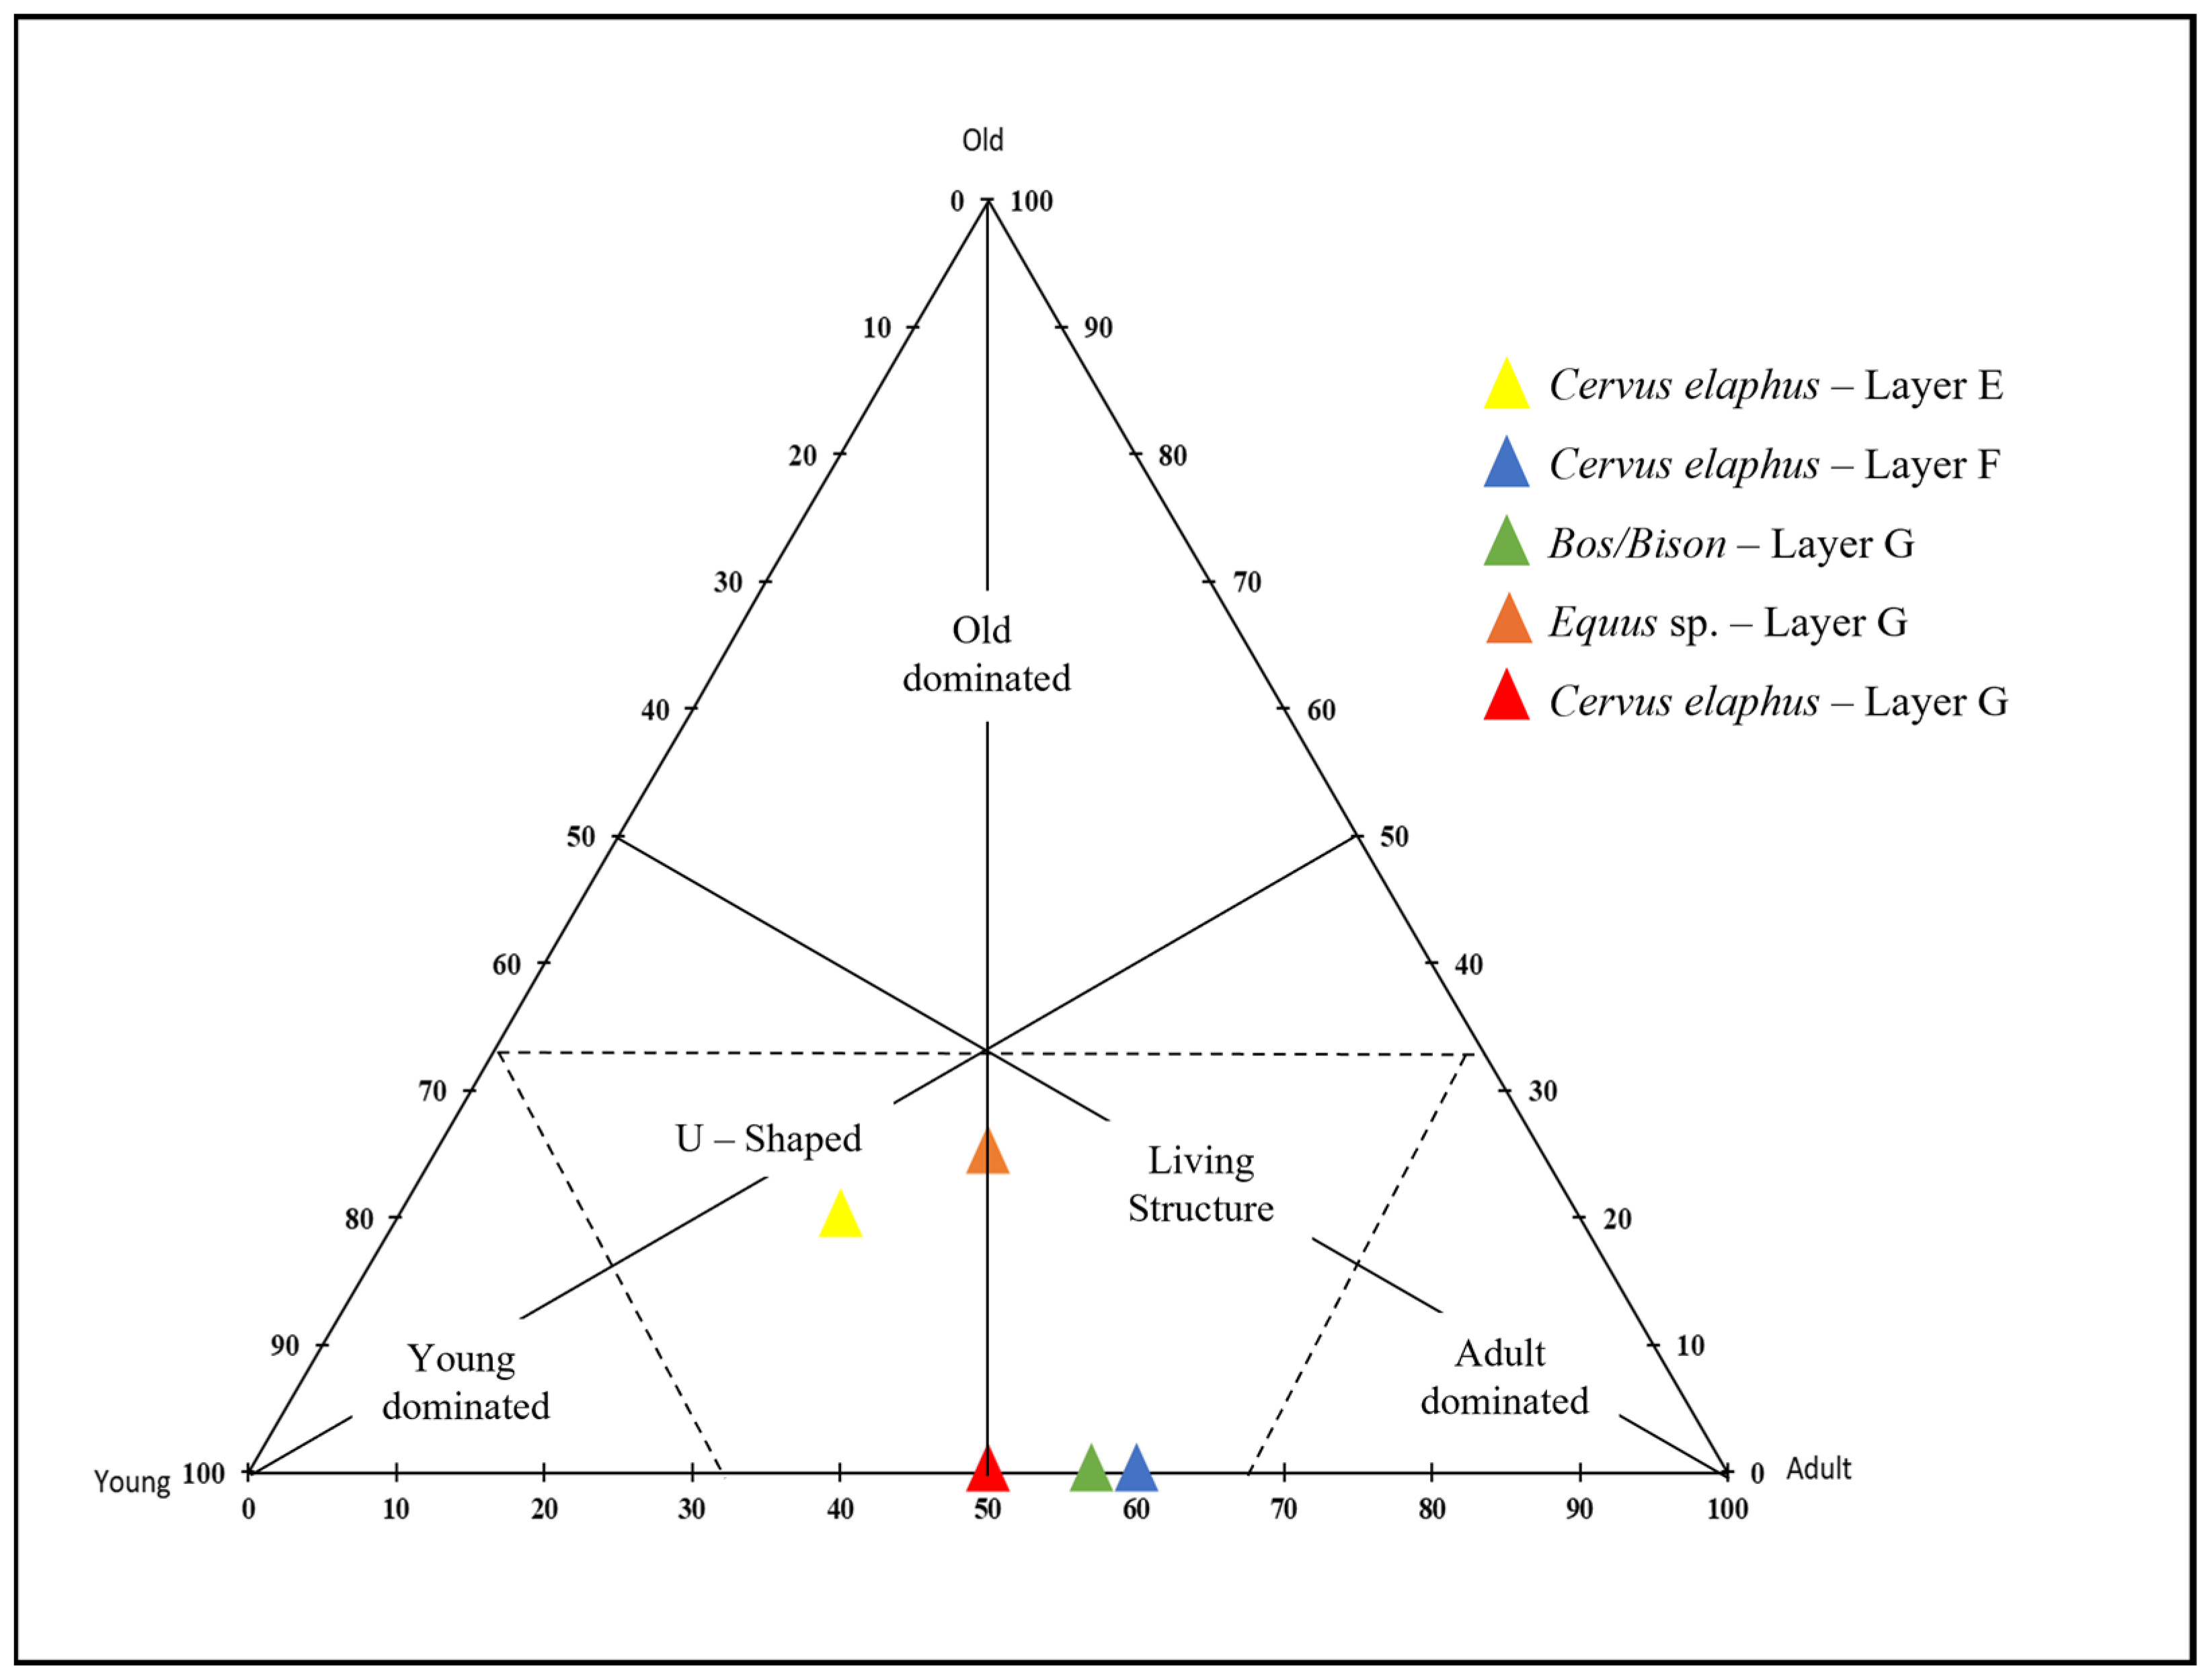
To evaluate species abundance, we considered the number of identified specimens (NISP), the minimum number of individuals (MNI), the minimum number of elements (MNE), and the standardised minimal animal units (MAU) [76,77,78]. For the quantification of the long bones, the coding method established by Romandini [79] after Marean et al. [80] was followed. Animal age at death was determined by examining dental eruption and wear and assessing bone fusion, following Silver’s established criteria [81]. For cervids, we applied species-specific ageing frameworks [82,83,84,85]. Caprids and bovids were analysed using known criteria from Couturier [86], Habermehl [87,88] and Pflieger [89] and equids have been classified following the Fernandez and Legendre [90] protocol. Leporids were classified using Broekhuizen and Maaskamp [91], Gardeisen and Valenzuela [92] and Jones [93]. After establishing the age at death, each individual was assigned to one of five age categories: F/NB (foetal/new born); J (juvenile—characterized by light wear on deciduous teeth and eruption of the first molar, M1); SAd (subadult—showing moderate wear on deciduous teeth and eruption of the second molar, M2); Ad (adult—with all permanent teeth erupted and exhibiting light to moderate wear); and S (senile/old adult—marked by advanced dental wear). Age-at-death analyses were investigated through ternary diagrams showing the proportions of senile, adult, and young individuals for the most abundant ungulate taxa in each stratigraphic layer [94,95]; only taxa with a minimum number of individuals (MNI) greater than 4 per layer were considered.
To evaluate transport strategies and attrition processes, the correlation between %MAU and bone density was calculated only in layer G for large bovids (Bos/Bison) and cervids (Cervus elaphus and Dama dama), the most abundant species in the assemblage. In addition, to assess the exploitation strategies, %MAU of ungulates was also correlated with other utility indices, such as the Modified General Utility Index (MGUI; [96]), MAX density, the Food Utility Index (FUI; [97]), the Meat Grease and Marrow Indexes, and the Unsaturated Marrow Index (UMI; [98]). For all of them, Spearman’s and Pearson’s correlation coefficients were calculated using PAST [99]. Assemblage diversity was examined using the Inverse of Simpson’s Index (1/D) with an MNI [100]. The higher the value (starting from 1), the wider the diet breadth [101].

3.2. Taphonomic Analysis

The bone surface of every specimen over 3 cm long was examined under a Leica S9i stereomicroscope (0.75–70× magnification range, Leica Microsystems, Wetzlar, Germany) and a Hirox HR-2016 3d digital microscope (Hirox Co., Ltd., Tokyo, Japan) to identify biostratinomic and diagenetic alterations. Evidence of anthropogenic modification observed on the faunal remains includes cutmarks, intentional bone breakage and burning [102,103,104,105,106]. Cutmarks (incisions and scraping marks) have been identified and recorded considering the following characteristics for each bone specimen: quantity, location, distribution (isolated, clustered or crossed), and orientation (longitudinal, transverse and oblique) on the bone surface. Moreover, to determine specific butchering activities (skinning, evisceration, dismemberment, defleshing, periosteum removal, and tendon cutting), experimental and ethnological studies on medium/large prey were used [27,102,107,108,109,110,111,112,113]. Intentional bone breakage was inferred from type and angle of fracturing (fresh-green versus old-dry) following Villa and Mahieu [114], and percussion marks, such as cortical percussion notches (negative flake scars), impact flakes (positive flake scars), adhering flakes, percussion pits and crushing marks [109,115,116,117,118,119,120,121,122]. As for impact flakes, the distinction from those made by carnivores was made following Coil et al. [123]. Burning damage was recorded based on presence/absence (macroscopically) and assessed using a modified version of the criteria described by Stiner et al. [124].
Carnivore-induced modifications were identified by diagnostic features, such as pits, scores, punctures, furrowing, gnawing, crenulated edges, and evidence of gastric acid etching. These were classified following the criteria established by Blumenschine [125], Domínguez-Rodrigo and Piqueras [126], and Domínguez-Rodrigo and Barba [127]. Additionally, a range of other biotic and abiotic surface alterations was recorded [128], including weathering [129], root etching, insect or fungal damage, carbonate encrustations, polishing [78,105,108], and the development of mineral coatings, particularly manganese oxides [128]. To distinguish trampling-induced modifications from anthropogenic cut marks, diagnostic criteria proposed by Blasco et al. [130] and Domínguez-Rodrigo et al. [131] were applied.

3.3. ZooMS Analysis and Glutamine Deamidation

A total of 24 bone specimens were sampled and analysed at the Palaeoproteomics Laboratory of the Bones Lab (Department of Cultural Heritage, University of Bologna, Ravenna) for ZooMS identification. Approximately 30–50 mg of bone was sampled. Collagen extraction followed the protocol established by Buckley et al. [132]. Samples were demineralised in 0.6 M HCl (hydrochloric acid) and subsequently incubated in ammonium bicarbonate (AmBic). The resulting supernatant was collected for trypsin digestion, after which the tryptic digests were purified and concentrated using in-house STAGE tips (Empore™). Following peptide elution, samples were dried overnight under a hood, then resuspended and sonicated. A matrix of α-cyano-4-hydroxycinnamic acid (CHCA, 10 mg/mL Sigma- Aldrich, St. Louis, MO, USA) was prepared, and for each sample, 1 µL of matrix was mixed with 1 µL of sample directly on a ground-steel target plate and allowed to air dry. Each specimen was spotted in duplicate. Analyses were performed using an Autoflex maX MALDI-TOF mass spectrometer (Bruker, Billerica, MA, USA), calibrated at regular intervals throughout the analytical session.
Spectra, each acquired from 3000 to 5000 laser shots, were manually inspected and averaged using mMass [133], after setting a signal-to-noise ratio equal to 3.5, a baseline correction and smoothing with the default parameters (baseline correction precision 100 and relative offset 0; smoothing method Savitzky–Golay algorithm, window size 0.2 m/z and 1.5 cycles; peak picking with deisotoping tool, relative intensity threshold 0.5% and picking height 80%) [134]. Taxonomic identification was carried out manually by comparing collagen peptide markers with reference spectra from Pleistocene and Holocene medium- to large-sized mammals [135,136,137,138].
Deamidation ratios were calculated for all the analysed samples. It is represented by a number ranging from 0 to 1, with 0 corresponding to complete deamidation and 1 representing a non-deamidated peptide. Deamidation of glutamine and asparagine residues is a common, non-enzymatic modification resulting in a +0.98402 mass shift caused by the conversion of a side-chain amide group to a carboxylate via a cyclic intermediate (glutarimide/succinimide) under alkaline and neutral conditions or direct hydrolysis under acidic conditions (or in the presence of metal cationic species) [139]. Peptides with m/z values of 1105.6 and 1706.7 were selected to determine the percentage of deamidation [139] using the R 4.0.1 q2e package [140].

4. Results

4.1. Taxonomic Composition

In total, the analysed assemblage comprises 2810 remains, distributed unevenly across the three layers under study: 968 from layer E, 380 from layer F and 1462 from layer G (Table 2; Figure 3; Figure S1). Sixty percent were identifiable to taxa, 2% to mammal body sizes and the remaining 38% were indeterminate fragments. The faunal assemblage comprises 3 vertebrate classes (Mammalia, Reptilia and Aves), with 16 species distributed across 17 genera. Mammals are represented by four orders (Lagomorpha, Carnivora, Perissodactyla, and Artiodactyla) and reptiles by chelonians; for birds, taxonomic identification did not proceed below the class level. Due to the fragmented state of the assemblages, a minimum number of elements (MNE) of 412 was quantified and a total MNI of 111, with adults predominant (Table 2).
Among the ungulates, Cervus elaphus represents the most abundant taxon across the assemblage and dominates layers E and F, while Dama dama is consistently represented in both levels. Equids are particularly abundant in layer F, whereas other ungulates, including Bos/Bison, Sus scrofa and Capreolus capreolus, occur in low proportions. Layer G shows a markedly different taxonomic composition, being dominated by birds and lagomorphs, while ungulates represent a minor component and are restricted to Bos/Bison and cervids (C. elaphus and D. dama). Other ungulate taxa have a scarce impact on the assemblage.
Among carnivores, remains are scattered. Vulpes vulpes is the most common taxon and is present in all three layers, with its highest abundance in layer E. The same layer also includes isolated remains of Canis lupus, Crocuta spelaea and Martes sp. In contrast, layer G shows a slightly higher taxonomic diversity among carnivores, with the occurrence of Panthera pardus, Lynx lynx and Meles meles, although each taxon is represented by one or two specimens only and does not affect the overall faunal composition.

4.2. Age-at-Death, Seasonality and Sex Determinations

As shown in Table 2, the three layers are dominated by adult individuals. Ungulates in layers E and F show comparable age structures dominated by adults, with a minor contribution of juvenile and senile individuals, whereas layer G displays a more diversified profile including foetal/newborn, juvenile, and adult individuals, with rare senile specimens. Carnivores are represented by very low MNI values in all layers and are almost exclusively composed of adult individuals, with no evident age structuring. Lagomorphs are negligible in layers E and F but show a marked increase in layer G, where the assemblage is dominated by adult individuals with a limited juvenile component. Testudo hermanni is recorded only in layer G and is represented by one juvenile specimen among all adults.
To further explore the age structure of the most abundant ungulate taxa, a ternary plot was constructed based on the proportions of senile, adult, and young individuals in each stratigraphic layer (Figure 4). Only taxa with an MNI > 4 per layer were included. Cervus elaphus, represented above this threshold in all layers, shows variable age structures, ranging from a relatively balanced profile in layer E to assemblages dominated by adults and young individuals in layers F and G, with senile individuals absent in the latter. Bos/Bison and Equus sp. exceed the inclusion threshold only in layer G. Bos/Bison is characterised by a dominance of adults and young individuals, whereas Equus sp. displays a more heterogeneous profile, including senile individuals.
Seasonality can be tentatively inferred from the presence of very young individuals. Two foetal/newborn cervids (one Cervus elaphus and one Dama dama) suggest mortality between summer and late autumn, while a juvenile Bos primigenius mandible with dp2–dp4 present and the first molar erupting, estimated at approximately six months of age, indicates death in early winter. Although based on a limited sample, these observations point to repeated or prolonged site use from early summer through early winter.
Regarding sex determination, it was only possible to infer the presence of a Cervus elaphus male specimen in layer G, where two antler fragments (MNE = 1) were recovered.

4.3. Taphonomic Observations

The bone assemblage shows very high fragmentation in layers E and F, where complete skeletal elements represent only 1% (N = 7 and 5, respectively), consisting primarily of teeth and compact bones, such as phalanges, carpals, tarsals, and sesamoids. In layer G, the proportion of complete elements rises to 15% (N = 218), reflecting the dominance of small game (lagomorphs, chelonians, and birds) whose small, compact bones are less prone to fragmentation than those of larger animals (Table S1). The high fragmentation observed in layers E and F may be related to the collapse of the cave roof, which would have left the remains exposed to weathering. However, more intensive exploitation of prey cannot be ruled out.
Low-density axial elements (ribs, sternum, and vertebrae) and girdle bones (shoulder and pelvic) are virtually absent in layer E and scarce in layer F (2%), likely due to their poor preservation potential. In layer G, however, fragmented remains of these elements reach 11%, a proportion largely driven by chelonian shell elements, which, despite being classified as axial elements, are considerably more resistant to fragmentation and destruction than other low-density bones (Table S1). In contrast, long bone shaft fragments are abundant (E = 5%; F = 14%; G = 10%; Table S1). Epiphyses, spongy, and flat bones are consistently underrepresented across all layers, with the lowest values recorded in layers E and F and virtually absent in layer G (Table S1).
Overall, the bone assemblage shows generally good preservation, with post-depositional fractures representing less than 10% of the total across all layers, though more frequent in layer G (Table S1). Fresh fractures are very limited in layers E and F (<1% and 2%, respectively), but more common in layer G (12%). Green breakage was generally identified on long bones and metapodials (Table S2).
Anthropogenic modifications were identified exclusively on faunal remains from layers E and G (Table 3), including butchery marks (cutmarks and intentional bone breakage) and evidence of thermal alteration (TA). Cutmarks (CM) and percussion marks (PM) were analysed according to their distribution, orientation, and morphology to identify butchering activities. The recorded marks primarily consist of short incisions associated with skinning, defleshing, and periosteum removal, along with scraping marks related to periosteum stripping and deep striae mainly associated with tendon extraction. Anthropogenic bone breakage was inferred from two types of percussion-related traces: impact notches and flakes.
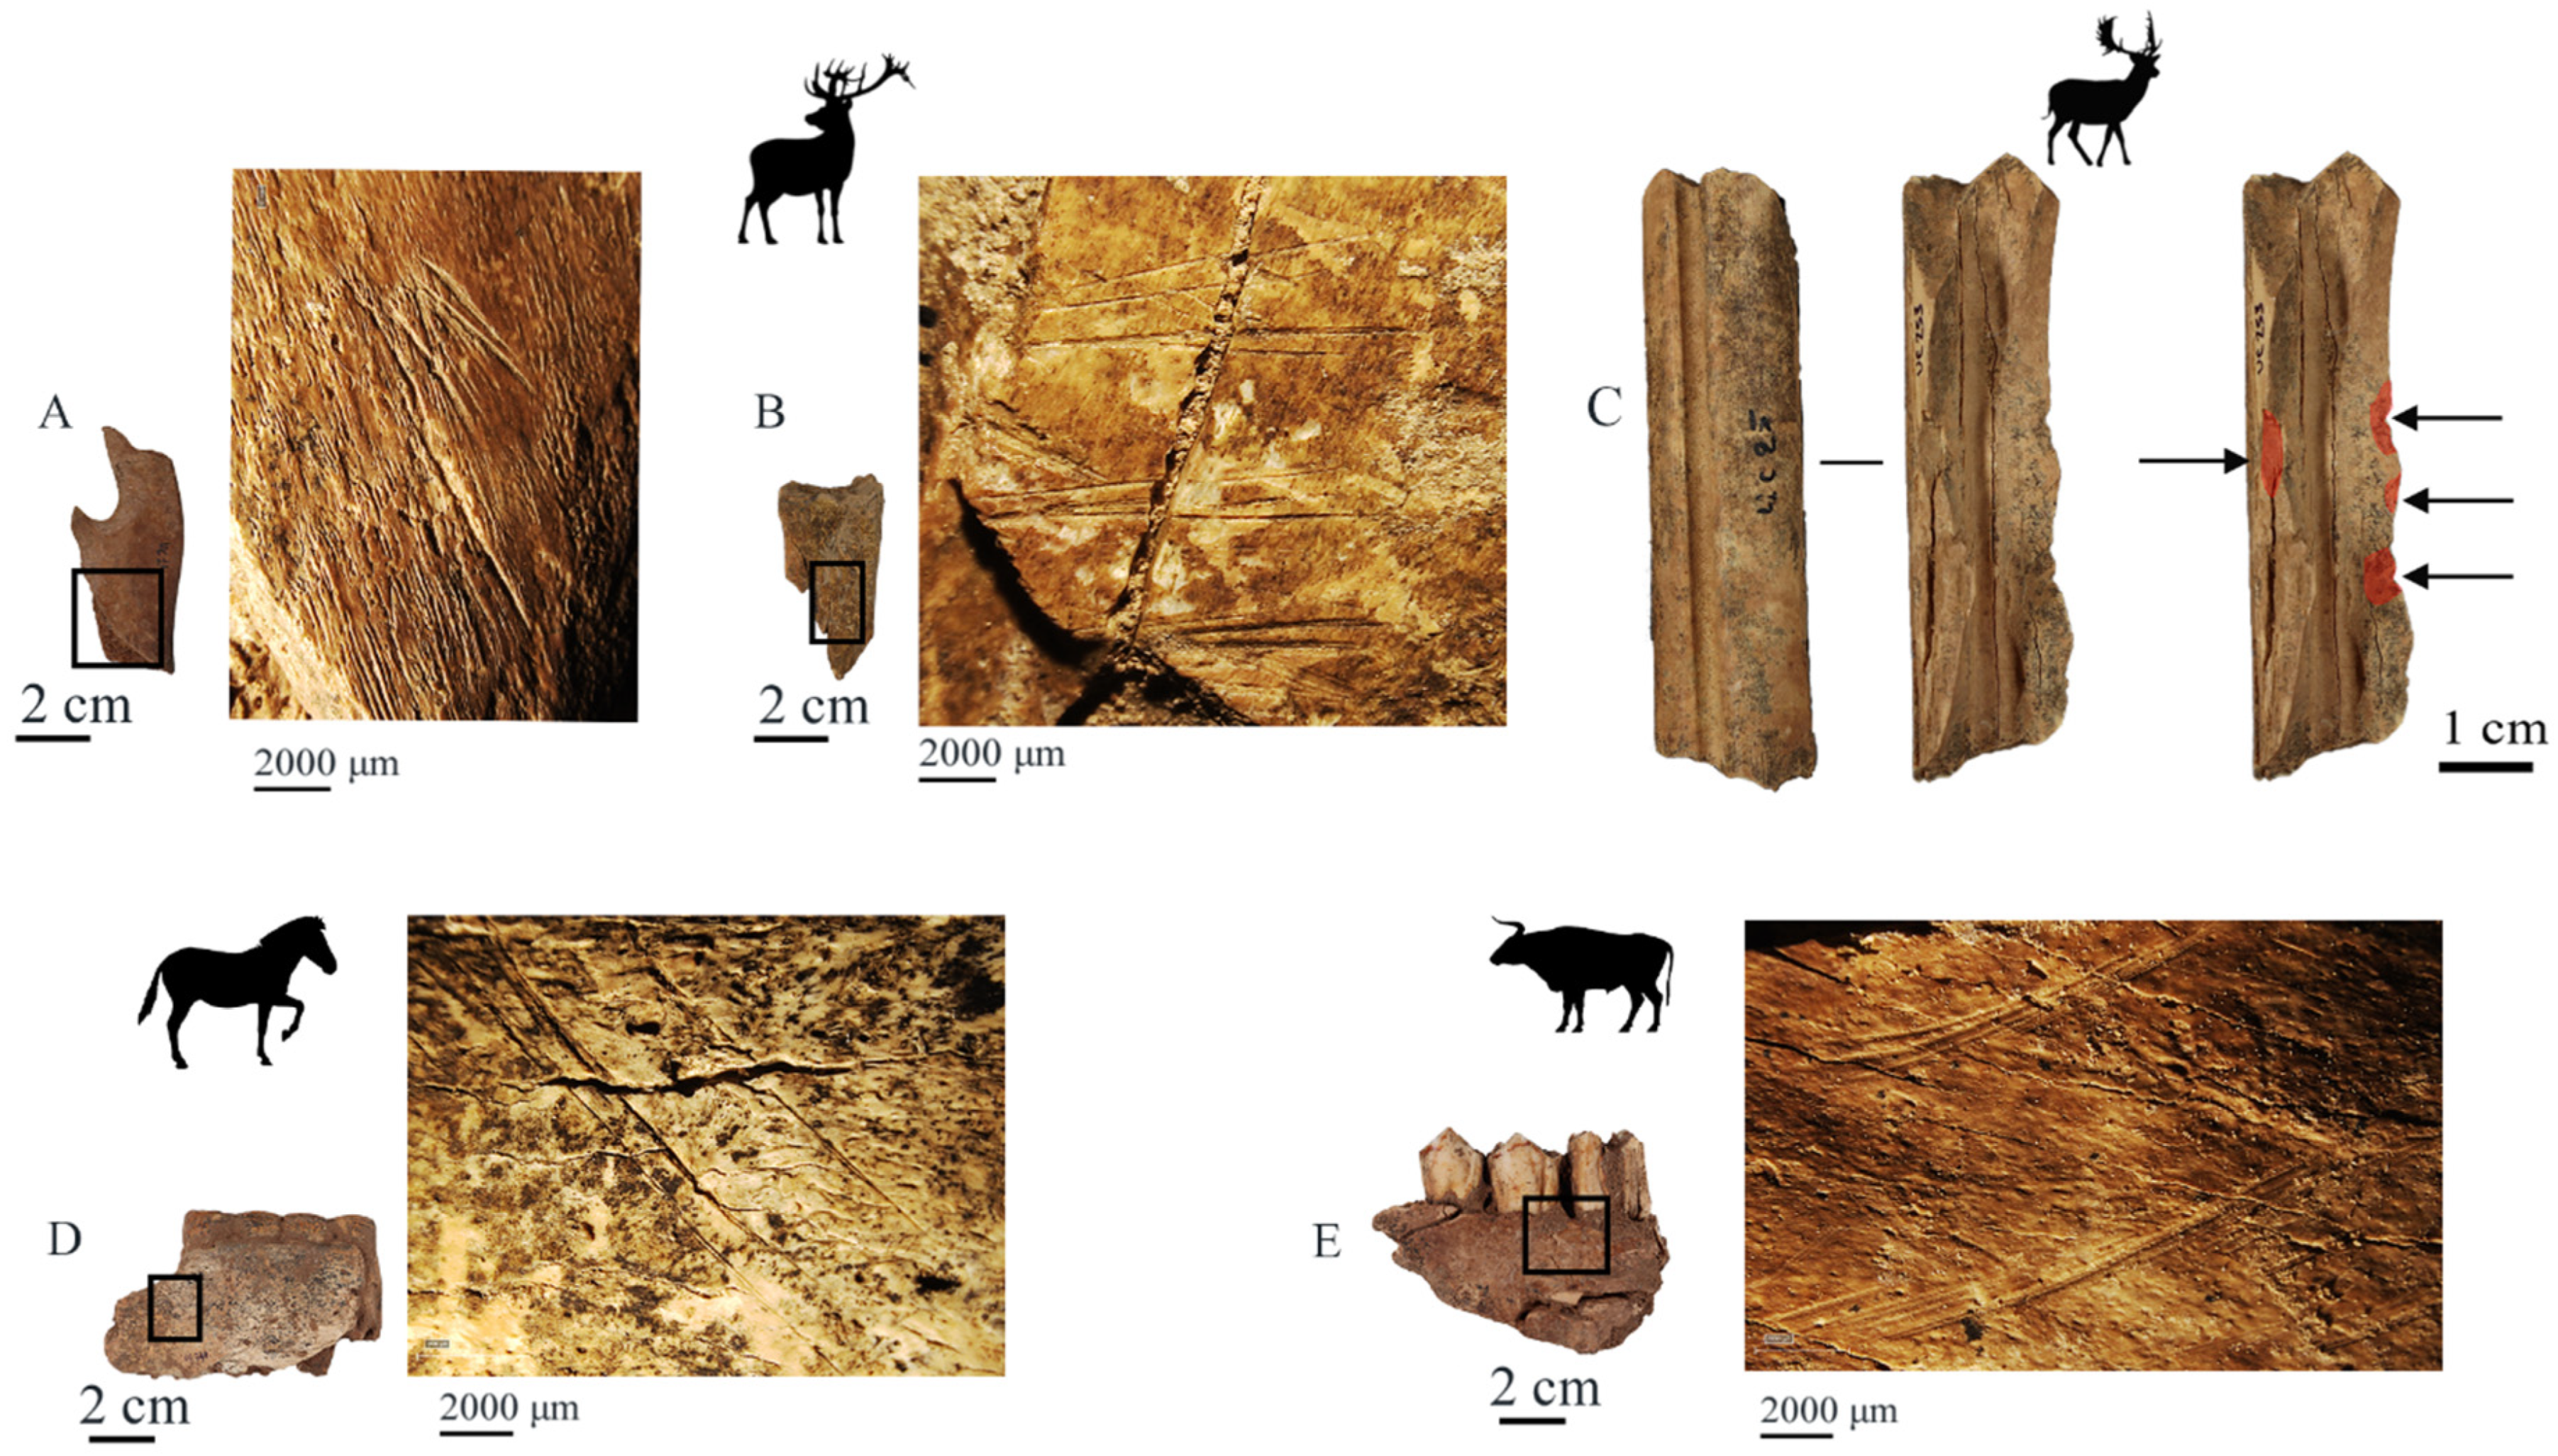
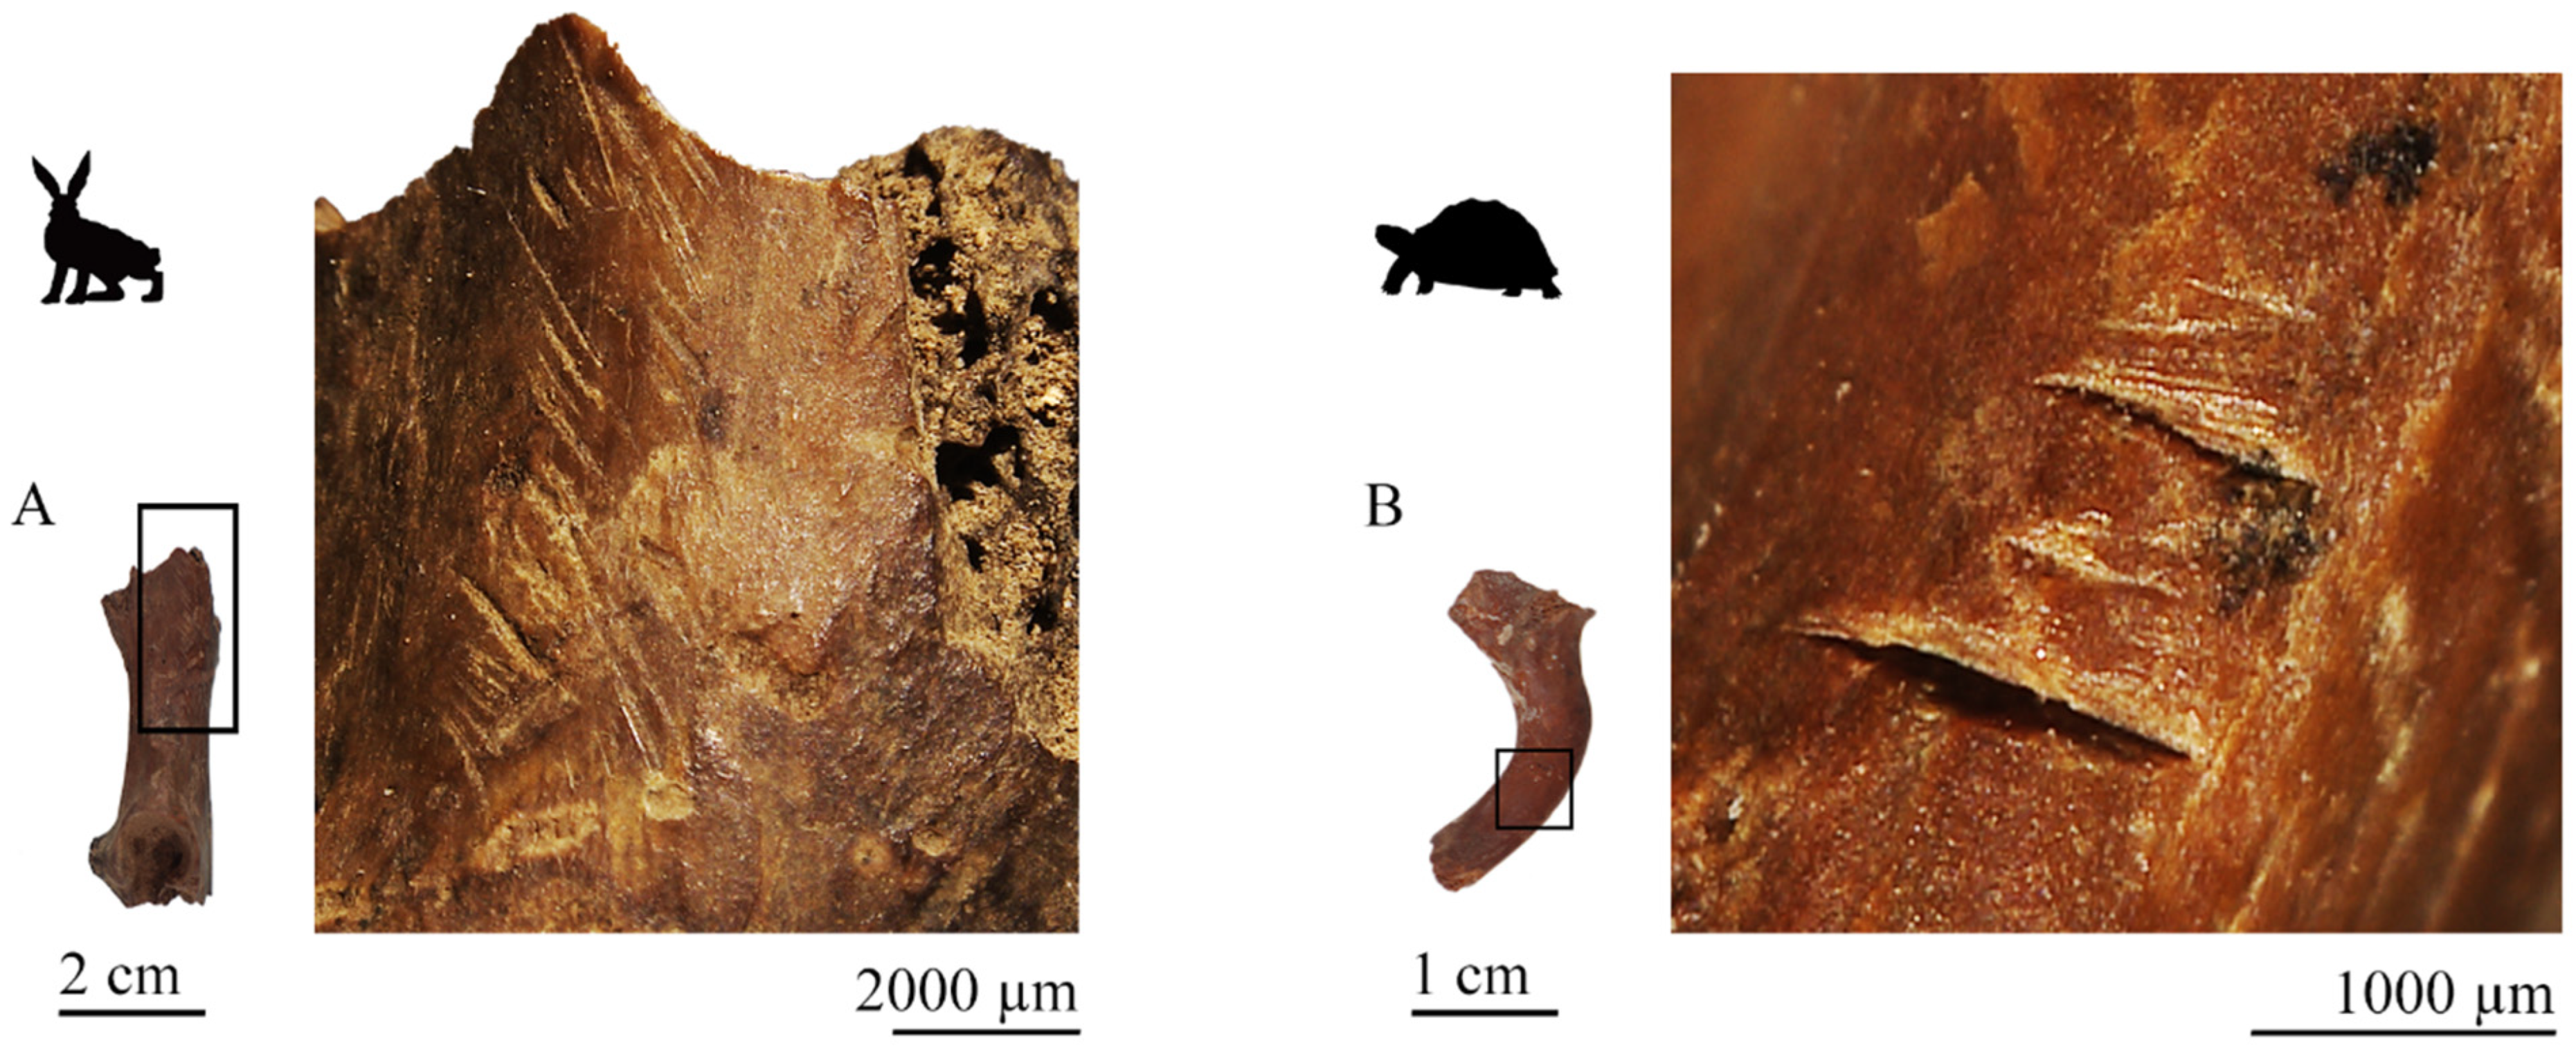
In layer E, cutmarks were recorded on one red deer tibial shaft (%BM = 5.6) and on one flat bone of an indeterminate mammal. In layer G, cutmarks were observed on ungulates, leporids, and chelonids. Among ungulate remains, two bones of large bovines (%BM = 1.1), one equid bone (%BM = 4.5), and two red deer bones (%BM = 5.7) show evidence of butchery. All three taxa exhibit multiple obliquely oriented incisions on the hemimandible. In B. primigenius and Equus sp., cutmarks are located on the medial surface just below the last premolar (dp3 in the case of Equus) and first molar, indicating mandible disarticulation and/or tongue removal (Figure 5D,E). The C. elaphus hemimandible shows cutmarks on the lateral surface beneath the condylar process, consistent with joint disarticulation or flesh removal (Figure 5A). The diaphysis of one Bos/Bison metatarsal bears multiple longitudinal incisions and oblique scraping marks associated with skinning and periosteum removal. Similarly, transverse incisions and deep striae were recorded on one red deer metatarsal near the proximal epiphysis (Figure 5B), suggesting hide removal and tendon extraction. Percussion marks include two flakes and one impact point on indeterminate remains from layer E, and one D. dama metatarsal with consecutive and opposite notches from layer G, all related to marrow extraction (Figure 5C). Among lagomorph remains, cutmarks were identified on nine bones: seven on Lepus sp. (%BM = 3) and two on indeterminate Lagomorpha (%BM = 1). These traces were distributed across nearly all anatomical districts, except for cranial and axial regions (Figure 6A). Regarding chelonians, cutmarks were recorded on eight bones (%BM = 7), predominantly on shell elements and humeri (Figure 6B).
Thermal alterations (Table 3) indicate a higher degree of combustion in layer G (10% of finds) than in layer E (5% of finds). In the uppermost layer, fire damage is limited to indeterminate remains and a single bone of an indeterminate ungulate (Figure S2A). In contrast, in layer G all ungulates, leporids and chelonians are affected by thermal alteration, together with a single specimen of L. lynx (Figure S2B). Fire damage is documented across all anatomical regions, including teeth, cranial fragments, small skeletal elements (such as phalanges and sesamoids) and chelonian shell elements. Overall, the degree of combustion is moderate; most of the affected specimens exhibit brown and/or black colouration, whereas only five calcined specimens (grey to white) were recorded, all originating from layer G.
Biostratinomic modifications are rare across all three stratigraphic units, affecting less than 5% of bone remains in each layer (Table 4). This pattern is consistent with relatively rapid burial and stable depositional environments. Evidence of carnivore activity is limited to isolated tooth marks (one in layer E, 17 in layer G) and digestion marks (two in layer E, five in layer F, and three in layer G). Rodent gnawing is similarly scarce (one in layer E, 21 in layer G). Weathering and trampling marks are infrequent (<1%) and occur only in layers E and G, while dermestid’s pupal chambers were recorded on a few remains from layer E (N= 3) and layer G (N= 7).
In contrast, diagenetic alterations are abundant throughout the bone assemblage and reflect notable variability in post-depositional processes across layers E, F, and G (Table 4). Concretions and manganese staining are the most frequent modifications, with concretions peaking in layer F (85%) and manganese oxide deposits most prominent in layer G (43%). These patterns likely reflect the specific microenvironmental conditions of Uluzzo C, interpreted as a karstic habitat where the sheltered setting promoted localised water percolation and mineral precipitation. Root etching is moderately represented, particularly in layer G (12%), suggesting periodic penetration of plant roots into the sediment, possibly facilitated by minor fissures in the overlying rock.
Despite the prevalence of mineral-related alterations, chemical weathering features, including corrosion, exfoliation, and water dissolution, occur at consistently low frequencies throughout the sequence (<1%). This pattern suggests that while the karst environment provided conditions conducive to mineral deposition through percolating groundwater, bones were sufficiently protected from prolonged subaerial exposure and aggressive chemical weathering, likely due to relatively rapid burial within the cave sediments.

4.4. Skeletal Profiles

Ungulates’ skeletal composition across the three layers is characterised by a significant presence of cranial elements, particularly isolated teeth, along with some fragmented parts of mandible, cranium and horn/antler (Table S3). In contrast, the axial skeleton is nearly absent, with few fragments of ribs and vertebrae from the three layers and two fragments of red deer sternum from layer G. The scarcity of post-cranial bones is more evident in layers E and F, whereas in layer G, skeletal profiles of both ungulates and carnivores are more complete.
As concerns main medium-large mammal taxa, the three layers show some differences in the distribution of forelimb, hindlimb, and extremities. Layer E is particularly poor, as red deer is only represented by one fragment of tibia, while the red fox skeletal profile only includes a few remains of fibula, metatarsal and phalanx II. In layer F, red deer are completely missing postcranial elements, whereas equids and fallow deer skeletons are better represented. Equids show some remains of limb bones (radius, carpals and metapodials) as well as phalanges (I and II), while fallow deer show more remains of the anterior extremity (humerus, radius and metacarpal) than the posterior (tibia and metatarsal). In layer G, post-cranial elements are more abundant and allow for more refined estimates of attrition processes and prey transport strategies.
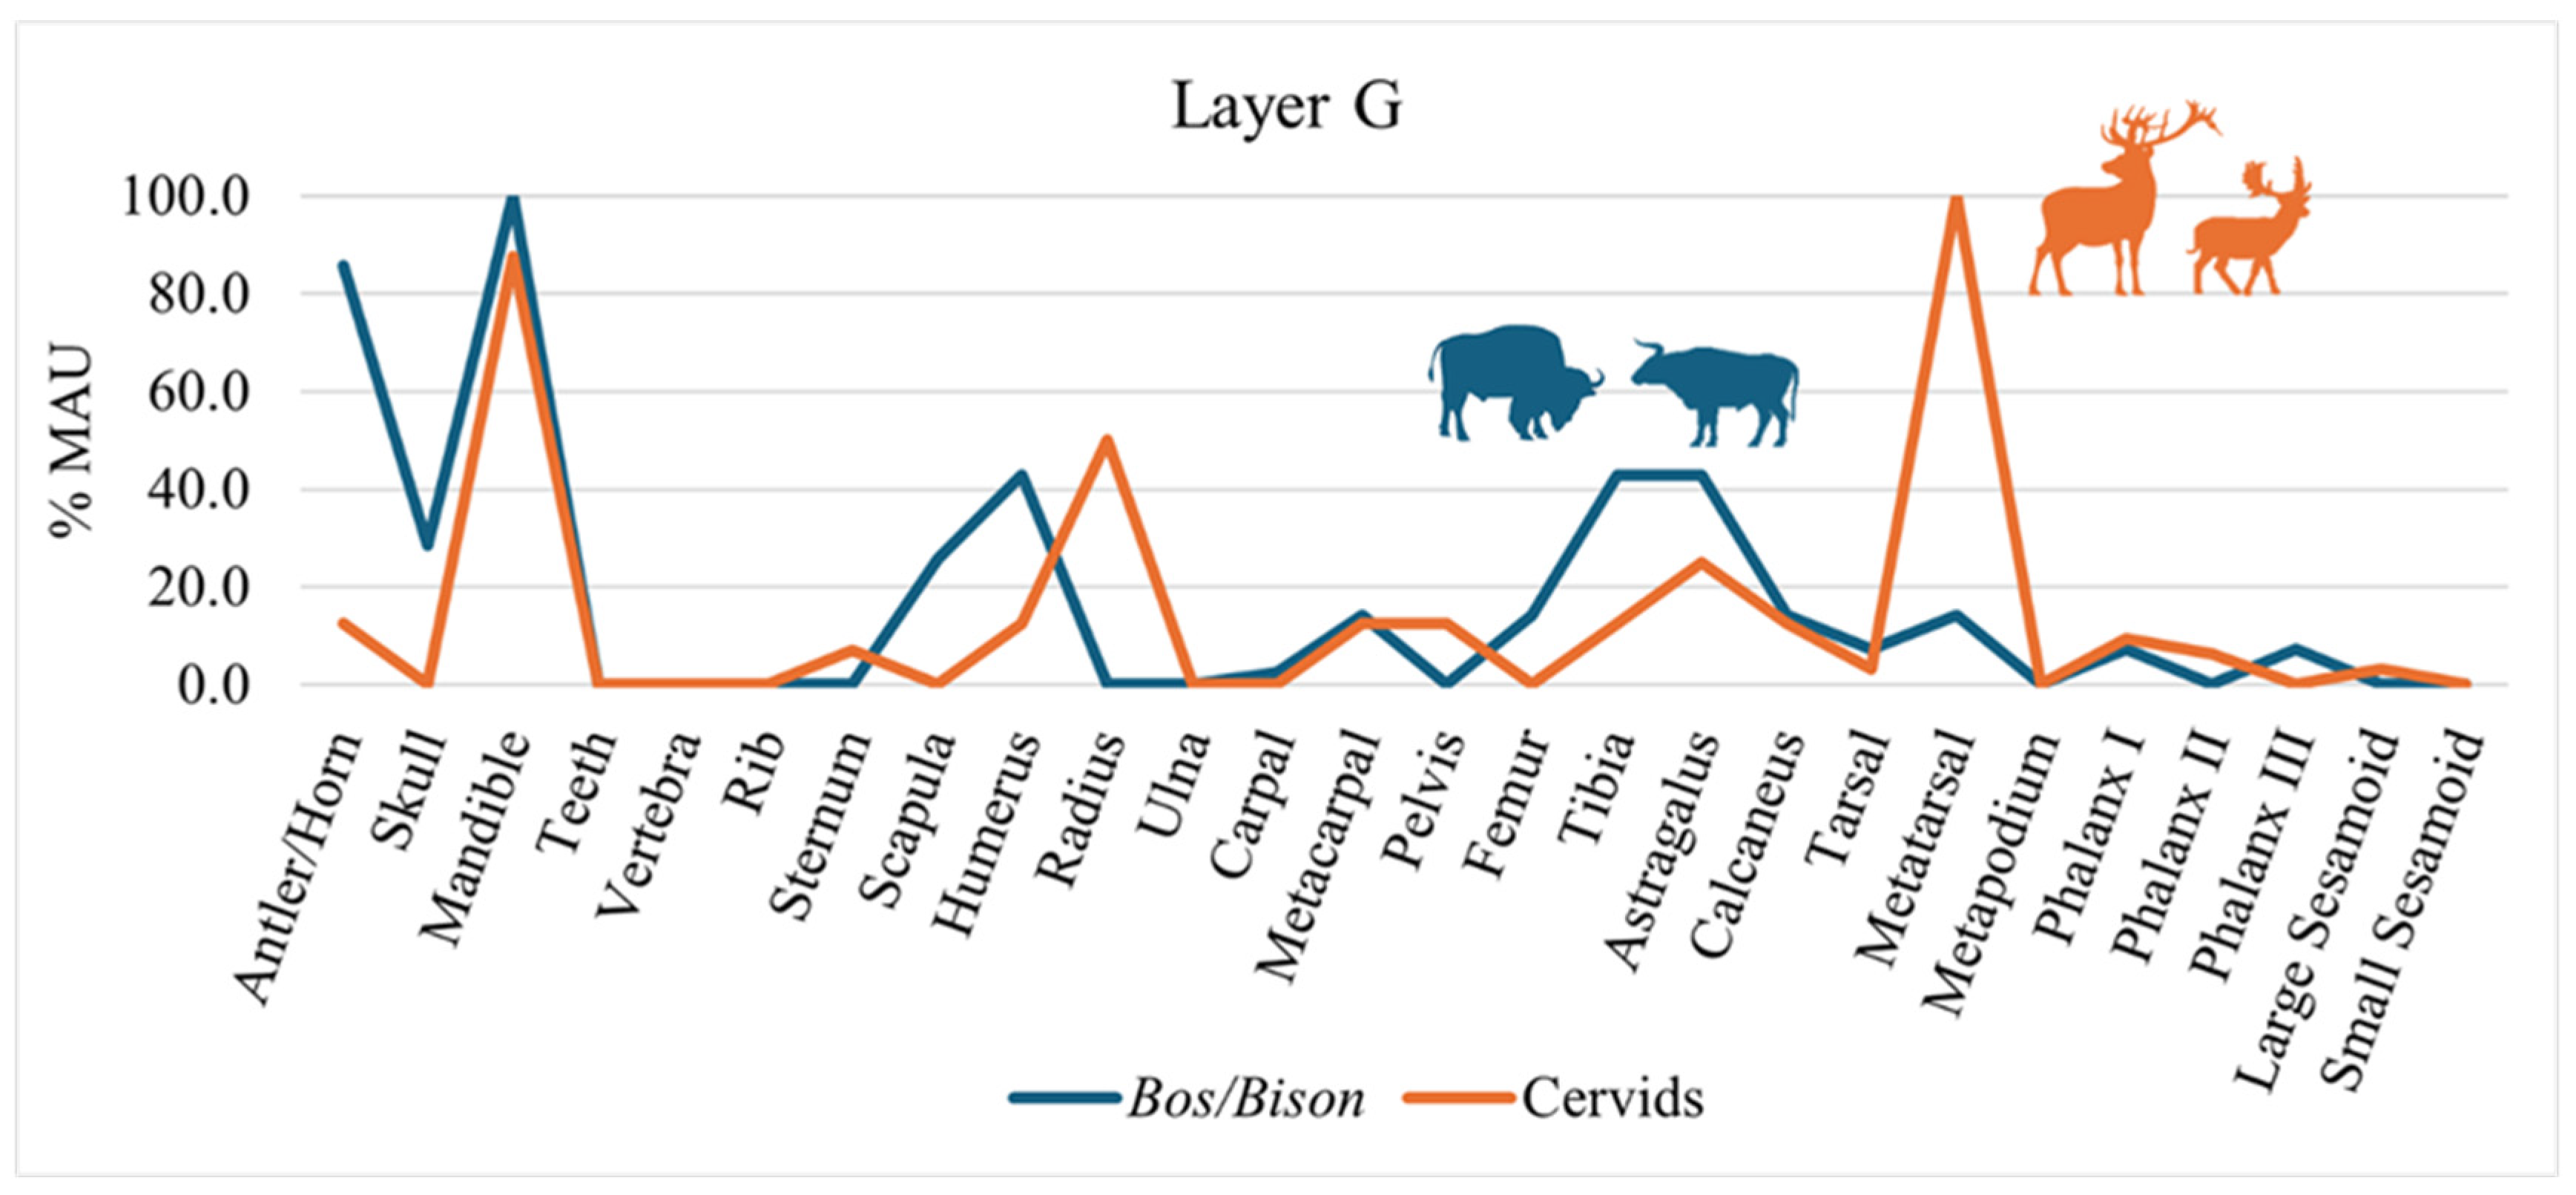
The large bovines (Bos/Bison) skeletal profile is mostly complete, as only a few elements are missing (i.e., radius, ulna and phalanx II). Based on NISP, the mandible (NISP = 12) stands out among cranial elements (excluding teeth) and horns (NISP = 6) are well represented. Likewise, in the appendicular skeleton, the most abundant elements are the tibia (NISP = 6), phalanx I (NISP = 5) and metatarsal (NISP = 4) (Table S3). The skeletal profile based on %MAU corroborates this pattern, with mandible and horn reaching the highest values (100% and 86%, respectively). Among post-cranial elements, humerus, tibia and astragalus display the highest %MAU values (43%) (Figure 7; Table S4). Correlation analysis between %MAU and the bone density for Bos/Bison shows no significant correlation (p > 0.05), nor are significant correlations found with utility indices (Table S5).
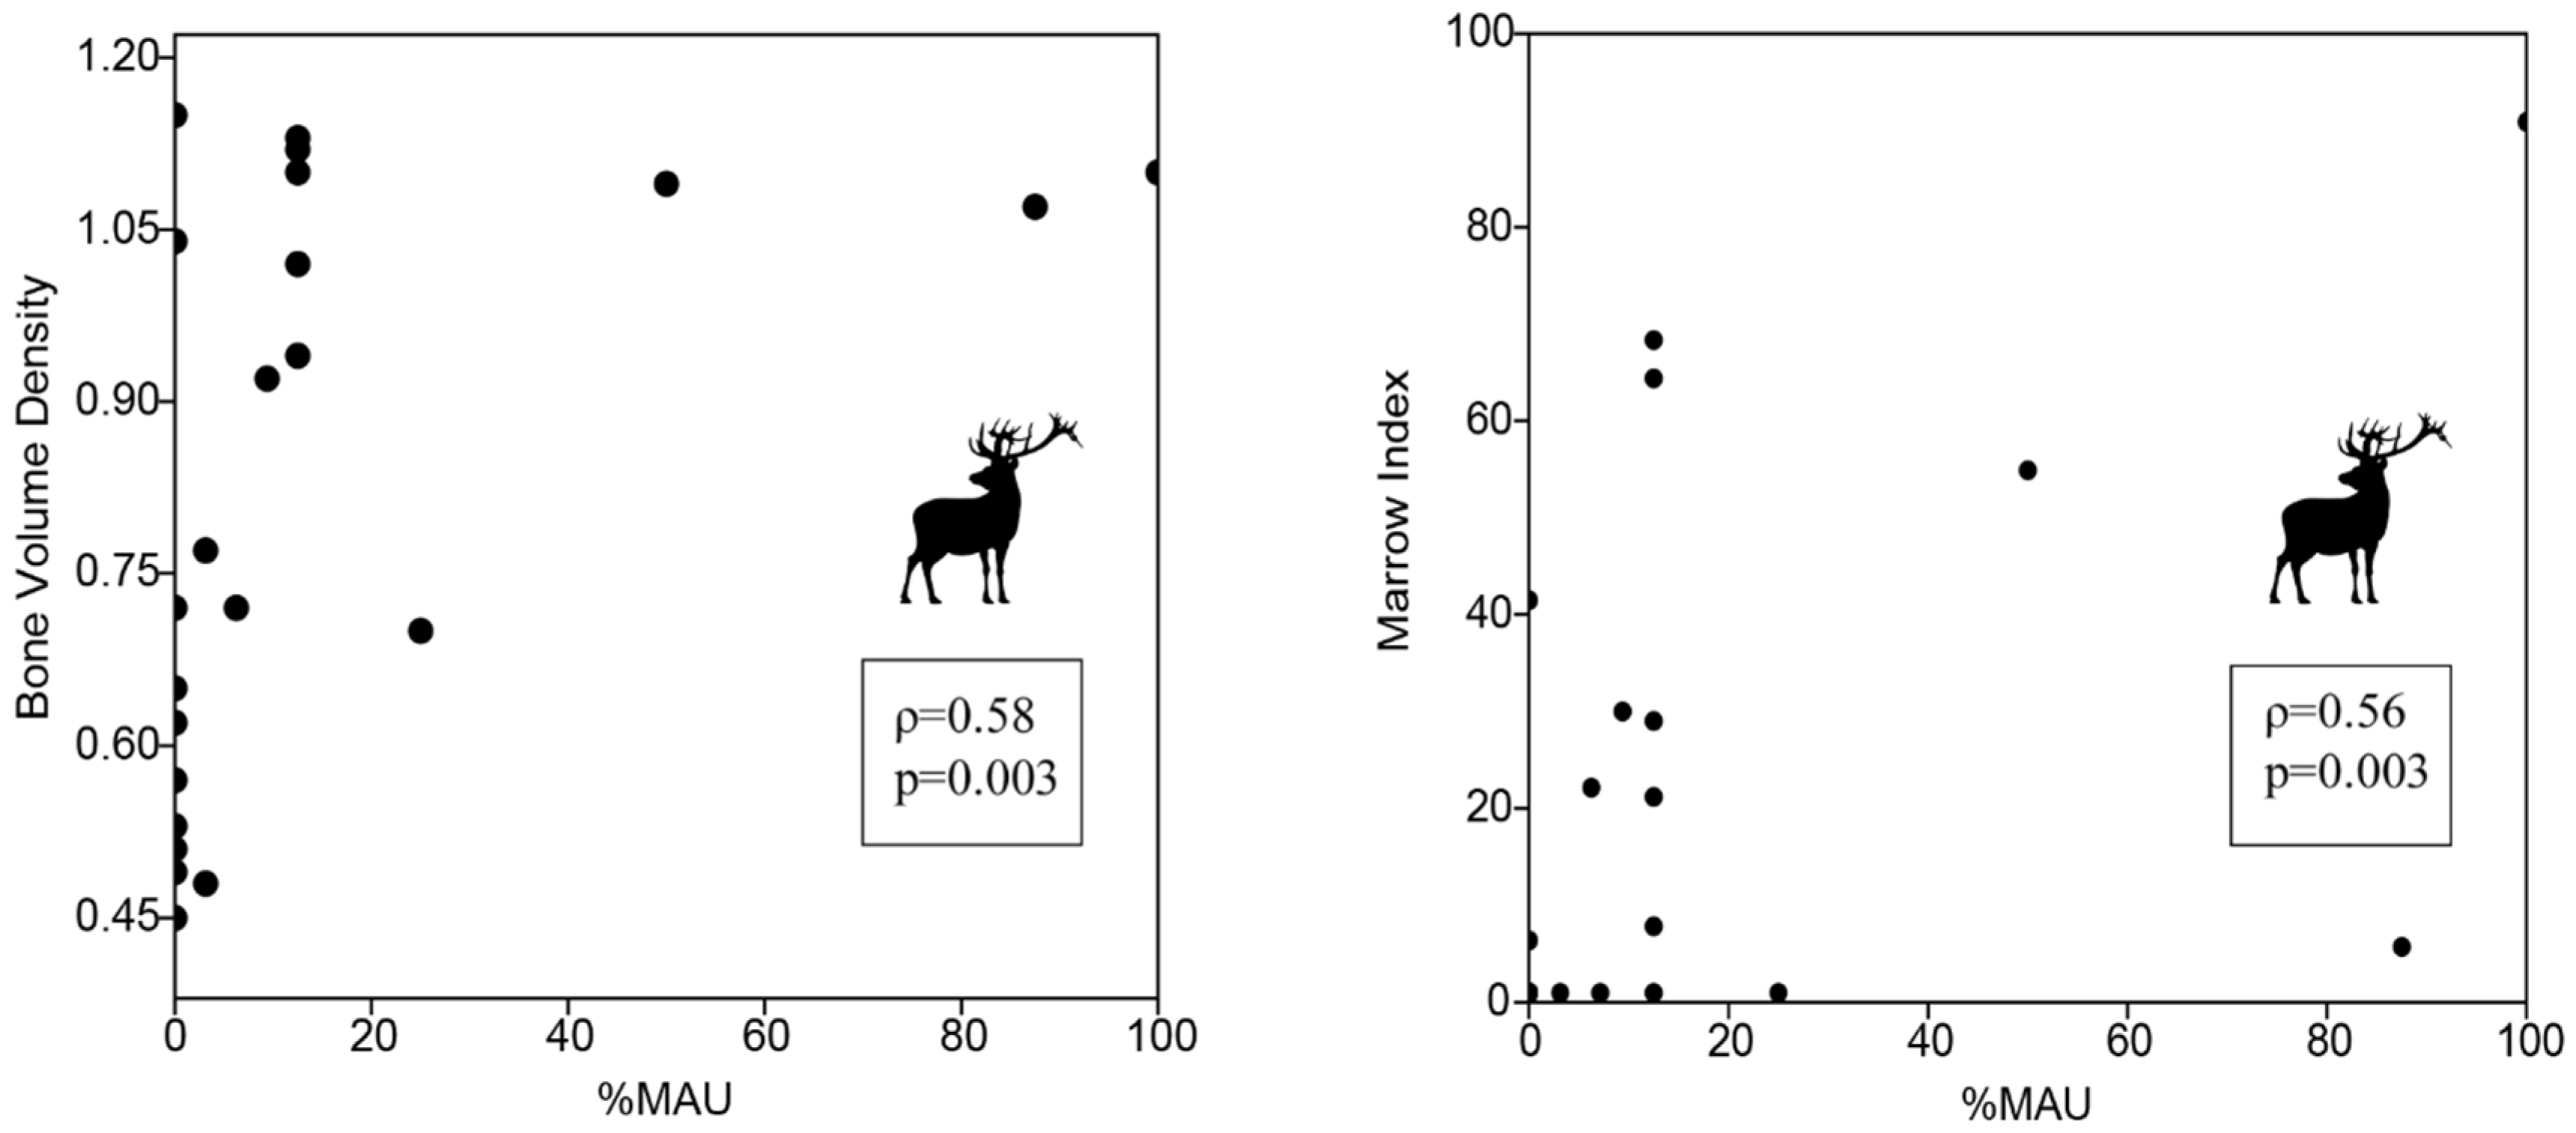
Regarding the remains of red deer and fallow deer from layer G, to increase statistical consistency, they were aggregated into a single category of medium-large cervids (NISP = 70) (Table S3). Although these are different genera, their similar size and bone morphology make density and utility indices comparable. The results should therefore be interpreted as indicative of exploitation strategies applied generically to medium-large cervids, without necessarily distinguishing between species. The cervid’s skeletal profile is generally complete, except for the absence of scapula, ulna, carpals, femur and phalanx III. According to NISP, the best represented post-cranial element is the metatarsal (NISP = 23), followed by the radius (NISP = 7) and phalanx I (NISP = 5), while in the cranial region, the mandible (NISP = 7) is the most abundant (not considering teeth). The %MAU profile shows a marked overrepresentation of metatarsal (100%) and mandible (87%), followed by radius (50%) and astragalus (25%), whereas phalanx I displays low values (<10%) (Figure 7, Table S4). Correlation analyses indicate statistically significant positive relationships between %MAU and several parameters (Table S5). A significant correlation is observed with bone density (ρ = 0.58; p = 0.003) (Figure 8). Significant positive correlations are also recorded with the Marrow Index (ρ = 0.56; p = 0.003) and UMI (ρ = 0.64; p = 0.017), while the correlation with the Grease Index approaches statistical significance (ρ = 0.40; p = 0.051) (Figure 8).

4.5. ZooMS Analysis

Out of the 24 samples analysed, only four obtained a taxonomic attribution, conferring a success rate of 16% (Table 5). One has been categorised as a possible human (Human? in Table 5) due to the presence of a single peptide associated with this species. However, given the very low spectral quality and the detection of only one human-specific peptide, this evidence is insufficient to support a reliable taxonomic determination. Further analyses, such as genetic investigations, are therefore required to achieve a secure identification of the fragment; for this reason, the sample has already been selected. The deamidation rates calculated for these samples are comprised between 0.26 and 1 for the peptide m/z 1105.57 and 0.07 and 0.42 for the peptide m/z 1706.77 (Figure S3). This wide range of values is contradictory to the low success rate obtained; further analysis would be required to identify the reason for such a gap.

5. Discussion

The palaeoenvironmental and zooarchaeological patterns documented at Uluzzo C must be interpreted in light of several factors that unevenly affect the number, preservation, and representativeness of the faunal remains across layers. Differences in specimen counts partly reflect post-depositional processes, including episodes of the vault collapse [58,65] that influenced both bone preservation and the visibility of surface modifications relevant for taphonomic analysis. In addition, the preliminary results of ZooMS analyses further support the interpretation that the local depositional context is unfavourable to organic preservation. The overall poor preservation of collagen in the samples is consistent with past analysis, which demonstrated that the pH of the sediment, the proximity of the sea (marine spray) and the average annual temperature of 17.6 °C explain the scarce preservation of the organic component at Uluzzo C [62,65]. Further uncertainty derives from the excavation history: because Borzatti did not provide a total count of the recovered faunal remains, it cannot be determined whether the material currently available corresponds to the entirety of what was originally excavated. Furthermore, the restricted horizontal exposure of the deposit, excavated primarily through narrow trenches, limits spatial comparability and may accentuate sampling biases. These constraints caution against overly fine-grained layer-by-layer comparisons and favour an interpretative framework centred on broader trends within the stratigraphic sequence. Nevertheless, despite these limitations, the assemblages preserve sufficient taxonomic and taphonomic information to support meaningful, although necessarily partial, palaeoecological and behavioural inferences. Ongoing excavations at the site will provide a more complete and spatially coherent record, allowing future research to confirm or revise these provisional interpretations.

5.1. Paleoenvironmental and Chronological Reconstruction of the Mousterian Layers

The taxonomic composition of the Mousterian sequence at Uluzzo C reflects dynamic environmental conditions and provides insight into the ecological and chronological framework of the site. Large bovids indicate the presence of open environments as well as wooded areas with clearings, typical of temperate conditions [141,142], while equids point to more extensive steppe and grassland environments under continental climatic regimes [141,142]. Cervids document a variety of wooded habitats, from dense forests for roe deer to Mediterranean scrub for fallow deer, with red deer, generally dominant in cold temperate phases, indicating the presence of mature forests [143]. Other taxa, such as wild boar, hare, rabbit, wolf, lynx and fox, are broadly adaptable and provide more limited palaeoecological resolution. Overall, the assemblage points to a heterogeneous mosaic landscape, combining open grasslands, woodland patches, Mediterranean vegetation and coastal wetlands.
Comparisons of the layers reveal subtle but significant ecological shifts (Figure S1). Layer E is dominated by C. elaphus, together with V. vulpes and D. dama, pointing to open woodland and ecotonal settings. Layer F, while still dominated by red deer, shows an increase in equids, indicating a more open grassland-forest mosaic. Layer G differs markedly, with abundant leporids and a significant representation of large bovids, alongside T. hermanni, pointing to increased openness, while maintaining temperate to warm-temperate niches suitable for tortoises.
Taxonomic diversity values further refine these interpretations. Layer E shows the highest Inverse Simpson’s Index (1/D = 6.67), reflecting a relatively heterogeneous faunal community typical of transitional ecotonal settings. Layer G exhibits similarly high diversity (1/D = 6.52), consistent with an open environment that nevertheless accommodated multiple ungulate taxa in comparable proportions. Layer F displays the lowest diversity (1/D = 4.26), which might suggest more ecologically constrained conditions dominated by a reduced suite of species.
The faunal evidence is supported by pollen data from layers E and F, which document a highly diverse and stable vegetation mosaic, including savannas with pine, oak, and juniper, steppe-like saltmarshes, riverine forest patches, open woodlands, shrubby grasslands with conifers and mesophytes, rocky scrub, grasslands with heaths and litoral vegetation [60]. These shifts outline a gradual transition from comparatively more closed and humid environments in layer E to increasingly open conditions in layers F and G.
The combination of taxonomic composition, species-specific climatic affinities, diversity patterns, and pollen data reinforces the view of Uluzzo C as a dynamic landscape, with each layer capturing a distinct yet complementary snapshot of paleoenvironmental variability. Compared with higher-latitude European contexts, the Italian peninsula, especially the south, maintained relatively mild conditions and high ecological diversity even during the cold stages of the Quaternary [144,145]. The proximity of the Ionian Sea at Uluzzo C likely helped moderate local climates, adding complexity to faunal patterns.
Most of the identified species have been present in Italy since the Middle Pleistocene, but the record also captures evolutionary and chronological dynamics. Modern forms of red deer and fallow deer are known only from the Late Pleistocene [146,147], while P. pardus, C. spelaea, and D. dama disappeared shortly before MIS 3 or during the Last Glacial Maximum. The latest occurrences of E. ferus date to the early Holocene, B. primigenius survived into historic times, and other taxa are still extant [143,148]. In Borzatti’s work [57], the presence of Rhinoceros mercki, currently referred to as Stephanorhinus kirchbergensis Jäger, 1839, was reported within layer G (spit 17), whereas no evidence of this taxon was identified in the present re-examination of the faunal record. Nevertheless, the possible occurrence of S. kirchbergensis would represent a highly significant palaeoecological and chronological indicator. This rhino is considered a grazer or mixed feeder, adapted to open environments and temperate to cold climatic conditions [149,150]. In the Italian and European record, the species is documented mainly during interpleniglacial phases of the late Middle Pleistocene, spanning from MIS 15 to MIS 5 [151,152]. Given that the base of layer G overlies a Tyrrhenian beach deposit attributed to MIS 5, its identification within layer G, and more specifically in spit 17, would therefore allow a considerable refinement of the chronological framework, support regional-scale stratigraphic correlations and contribute to a more precise reconstruction of the local paleoenvironment. Of chronological significance is the association of cave hyena in layers E and G with fallow deer, found across all layers. This combination firmly situates the sequence within a Late Pleistocene interval, between MIS 5 and MIS 3 [146,148]. Taken together, the palaeoecological and faunal patterns observed at Uluzzo C are fully compatible with the chronometric framework established with the OSL ages for the upper Mousterian units and the constraint provided by the PGT/Y-6 tephra [60,65], supporting a Mousterian occupation spanning from MIS 5 to late MIS 3.
A comparison between the Mousterian and Uluzzian layers at Uluzzo C highlights both continuity and significant ecological transformations, consistently reflected in the faunal and pollen records. The Uluzzian sequence (layers C and D; [63,64]) records a progressive environmental transition from relatively wooded and humid conditions to increasingly open and fragmented habitats. From a quantitative perspective, diversity metrics further underscore these shifts. Despite this, diversity values for the Uluzzian assemblage (1/D = 6.25) remain comparable to the most heterogeneous Mousterian layers, indicating sustained ecological complexity. This suggests that, despite the increasing openness of the landscape, the Uluzzian phases maintained a high degree of ecological heterogeneity, comparable to the more diversified Mousterian horizons and distinct from the more constrained conditions reflected in layer F.
In this context, Uluzzo C offers both a local picture of habitat changes and a representative example of broader regional palaeoecological dynamics during the late Middle Palaeolithic.

5.2. Uluzzo C Within the Apulian Mousterian Framework

Considering the Mousterian layers of Uluzzo C (E, F, and G) collectively, the faunal assemblage exhibits a consistent pattern of dominance by cervids, equids, and large bovids, reflecting the exploitation of heterogeneous landscapes that combine open areas with patches of woodland. When compared with coeval Mousterian sites across southern Italy, particularly in Apulia (Table S6), the Uluzzo C Mousterian sequence aligns closely with the ecological patterns documented at Grotta del Cavallo [153,154,155], Riparo l’Oscurusciuto [53,156,157], and Grotta Santa Croce [46,55,158], where cervids, equids, and aurochs dominate, indicating semi-open to open woodland environments. Broader consideration of other sites, including Grotta dei Giganti [159], Tana delle Iene [141], Grotta Romanelli [160,161,162,163], and Avetrana [142,164,165], reveals a consistent regional pattern: faunal assemblages frequently combine large bovids, cervids, and equids, reflecting heterogeneous landscapes that range from ecotonal woodlands and semi-open forests to more open, steppe-like habitats.
Zooarchaeological and taphonomic analyses demonstrate that bone accumulation at Uluzzo C was predominantly anthropogenic throughout the Mousterian sequence, as highlighted by diagnostic fracture patterns, butchery marks, and thermal modifications. These findings corroborate the evidence for human occupation already attested by the considerable lithic assemblage recovered throughout all levels, a production fully consistent with the Mousterian technocomplex documented across the Apulian region [56,166], as well as by the hearths identified in level G [58].
Nevertheless, the possible involvement of carnivores, particularly hyenas, warrants examination to assess their contribution to the assemblage. Borzatti already reported the presence of hyenas in layer G based on the recovery of coprolites [57]. In line with this, the faunal assemblage includes coprolites preliminarily attributed to cave hyena, currently under study, from layers E and G. In addition, fossil remains of cave hyena, including a mandible of a juvenile individual, have been recovered from the same layers (E and G). Despite the low frequency of carnivore tooth marks and other diagnostic modification traces (7 in the whole assemblage), the presence of coprolites and cave hyena remains suggests that the cave was used as a den, albeit sporadically, most likely when Neanderthal groups were elsewhere. Such alternating use of caves by humans and large carnivores is a well-documented pattern in Late Pleistocene contexts in Italy, including Grotta Paglicci [167], Grotta Guattari [168], Grotta del Fossellone and Grotta Breuil [169], Buca della Iena [170] and Grotta dei Santi [171] among others.
Within this framework, the limited impact of carnivore activity on bone surfaces at Uluzzo C may reflect short-term or episodic carnivore occupations rather than intensive carcass accumulation and processing. Overall, this integrated evidence provides a coherent framework for interpreting the formation processes and post-depositional history of the site assemblage, emphasising a predominantly anthropogenic origin of the deposit, with a secondary contribution from carnivore use of the site. Having established the predominantly human origin of the faunal assemblage, it becomes possible to reconstruct the subsistence strategies that drove its formation.
The results of this study may indicate that, in layers E and F, Neanderthal hunting strategies were primarily focused on medium- to large-sized ungulates, with a clear emphasis on large bovines, cervids, and equids. During the earlier occupational phase (layer G), human predation appears to have been more variable, spreading from large bovines and cervids to leporids and chelonians. A substantial presence of butchery marks and thermal alteration on small game remains show clear evidence of human consumption, demonstrating that small prey exploitation was part of Neanderthal behaviour at the site.
The Mousterian assemblage from Uluzzo C can be further contextualised within the broader framework of Middle Palaeolithic sites in Apulia, which show consistent patterns of resource exploitation and site use. Comparable strategies are documented at Riparo l’Oscurusciuto (Ginosa, Taranto), where high-utility portions of large ungulates were preferentially transported and intensively processed, and where lithic and faunal evidence suggest structured activity areas and repeated use of space for butchery and other tasks [53,156,157]. Similarly, Grotta del Cavallo (Nardò, Lecce) exhibits systematic butchery of cervids and other large ungulates, along with a persistent presence of anthropogenic modifications across multiple layers, reflecting repeated and structured Neanderthal occupations [54,154,155,172]. Grotta di Santa Croce (Bisceglie, Bari) further confirms these regional patterns, showing dominance of adult large ungulates, intensive bone breakage to access marrow and grease, and selective transport of high-utility skeletal elements [55,173,174,175].
When considered within a diachronic framework, the age-at-death patterns of the main prey taxa at Uluzzo C (Figure 4) can be discussed in relation to broader changes in Neanderthal hunting behaviour, while remaining mindful of the interpretative constraints imposed by the limited dataset. In the earliest occupation (layer G), the predominance of prime-age adults among large bovines and equids, together with the scarcity of old-adult individuals among red deer, may suggest some degree of selective exploitation of high-return prey. A similar pattern could be tentatively identified in layer F, where the apparent focus on prime adult red deer might reflect a continuation, or even a mild intensification, of such strategies. In the most recent occupation (layer E), however, the U-shaped mortality profile observed for red deer, characterised by an increased representation of juveniles and older individuals, may indicate a shift towards more vulnerable animals, possibly linked to changes in prey availability, hunting opportunities, or efficiency. Taken together, these patterns tentatively suggest a diachronic trend in prey selection strategies across the sequence, though the available evidence remains limited and alternative explanations cannot be ruled out.
When tentatively considered alongside preliminary indications of summer hunting activity, these demographic patterns could suggest a degree of forward planning that exploited seasonally predictable aspects of prey behaviour, such as migration routes or aggregation sites. However, it is important to emphasise that the seasonal signal within the assemblage remains ambiguous. The current evidence does not permit other periods of site occupation or hunting activity to be confidently excluded, nor does it establish a definitive seasonal focus. Both the mortality data and the seasonal indicators should therefore be regarded as suggestive of possible behavioural patterns rather than as conclusive demonstrations of planned seasonal hunting strategies.
Regarding carcass processing and transport strategies, several hypotheses may be advanced based on the available evidence. The skeletal representation of large ungulates across the Mousterian sequence is dominated by cranial remains, primarily teeth, with limb bones occurring less frequently and axial elements being extremely scarce. While dental survivorship partly reflects the superior durability of tooth enamel, the broader pattern suggests deliberate choices in which body parts were introduced to the site. Layer G, which yielded the most anatomically diverse assemblage, offers the clearest window into these transport behaviours, particularly for large bovids and cervids where sample sizes exceeded the threshold for meaningful statistical evaluation (MNE > 35).
For large bovids, the skeletal profile reveals a relatively complete representation of appendicular elements alongside a near-complete absence of axial bones and a marked underrepresentation of extremities. Although statistical tests between %MAU values and both bone mineral density and food utility indices failed to produce significant correlations, this may reflect the complex interplay of multiple formation processes rather than the absence of patterned behaviour. The profile itself, emphasising limbs and crania while excluding lower-value body portions, could tentatively suggest field butchery practices in which hunters may have prioritised the transport of meat-bearing and marrow-rich elements over bulkier, lower-yield axial portions.
Unlike large bovids, the cervids assemblage from layer G yields stronger statistical support for nutritionally driven transport strategies. While bone mineral density shows a significant positive correlation with skeletal part representation, indicating that attritional loss preferentially affected less robust elements, the assemblage also exhibits significant correlations with multiple food utility indices. The relationship is particularly pronounced for marrow values, suggesting that elements rich in this high-calorie resource may have been preferentially transported or retained. This is further supported by the presence of percussion marks indicative of marrow extraction, including anvil-assisted fracturing (Figure 5C). Weaker but still significant positive correlations with grease and general meat utility (UMI) indices also suggest that soft tissue exploitation may have played a role, a pattern tentatively corroborated by the presence of cutmarks. Such preferences would have been influenced by factors including prey body size, group composition, and the distance between kill and consumption locations. In this regard, the abundance of cranial remains at Uluzzo C warrants consideration in relation to ethnoarchaeological models linking head transport to group size and mobility [176,177]. The pattern at Uluzzo C, particularly in layer G, with a pronounced representation of cranial elements, implies that entire heads may have been transported rather than discarded during field processing. Therefore, if layer G represents occupations by groups large enough to manage the transport of heavy, lower-utility body parts, cranial abundance would align with reduced selectivity characteristic of larger aggregations [178]. Alternatively, heads may have been specifically targeted for secondary exploitation requiring controlled heat and time investment, such as brain extraction or rendering of cranial soft tissues [84,179]. Both scenarios imply a structured approach to carcass management and thermal processing strategies. The nature and intensity of such thermal processing can be further explored through the distribution and characteristics of fire-related bone modifications across the sequence.
Although not abundant, the proportion of thermally altered remains in layer G (10%) is nonetheless noteworthy, especially when compared to the uppermost Mousterian layers, among which only layer E yielded more limited evidence (5%) (Figure S2). Fire-related modifications are almost entirely of moderate intensity: charred bones dominate the thermally altered assemblage, while calcined specimens are virtually absent. This pattern closely resembles that documented for the Uluzzian layers at Uluzzo C, where 13% of faunal remains exhibit burning [62,63], but differs from other regional Mousterian sites, such as Grotta del Cavallo, Grotta Santa Croce, and Riparo l’Oscurusciuto, where thermally altered specimens account for less than 5% of their respective assemblages [55].
These differences reflect contrasting approaches to fire management and carcass processing across Apulian Neanderthal sites. At Oscurusciuto, despite the presence of multiple hearth features, bone remains show no evidence of having been used as fuel, leading researchers to attribute the scarcity of vertebrae and ribs to selective transport strategies rather than combustion-related destruction [157]. Conversely, at Grotta del Cavallo and Grotta Santa Croce, both interpreted as residential camps where intensive butchery activities took place, the low frequency of thermal alterations has been linked to systematic bone grease rendering. This inference rests on the combination of skeletal profiles dominated by high-utility elements, mortality patterns focused on prime adults, absence of carnivore modifications, and the minimal thermal alteration consistent with controlled, low-temperature heating required for grease extraction and exploitation, which seemed to have been particularly significant for Apulian Neanderthals [158].
Within this framework, Uluzzo C presents a more ambiguous picture. Like Oscurusciuto, the assemblage exhibits selective transport favouring crania and limbs, with no clear evidence that bone was systematically used as fuel. However, unlike the bone grease rendering scenario documented at Cavallo and Santa Croce, characterised by minimal thermal modification, layer G displays higher frequencies of moderate-intensity burning. This pattern does not align neatly with either model: the thermal alterations are too abundant to reflect dedicated low-temperature grease rendering, yet too moderate in intensity to suggest use of bone as primary fuel. The distribution and character of burning may instead point to incidental exposure during other cooking or heating activities, or to more varied fire-related processing practices than those documented elsewhere in the region.
It is worth noting that the combination of frequent, albeit moderate-intensity, thermal alterations, structured hearth features, and evidence for on-site marrow extraction points toward a residential occupation pattern. This interpretation is consistent with the hypothesis of Uluzzo C as a residential camp based on the lithic evidence, which records a complete chaîne opératoire [180]. Uluzzo Bay offered key advantages for repeated occupation, combining access to high-quality flint, with a plateau overlooking the bay suitable for hunting and foraging, where northern Ionian coastal sites, such as Uluzzo C and Grotta del Cavallo, were used as prolonged residential bases, while southern locations fulfilled more specialised logistical roles [180]. In addition, skeletal part representation and butchery trace frequencies may indicate selective transport of high-utility elements and limited on-site primary carcass processing. The low frequency of axial elements and extremities implies that the early stages of carcass dismemberment may have taken place elsewhere in the landscape, with only selected portions brought into the cave for final consumption and marrow extraction. This pattern likely reflects logistical decisions related to prey body size, kill-site distance, and mobility constraints, suggesting that even residential bases functioned within a broader spatial framework in which different stages of carcass processing were distributed across multiple locations. When considered together, the lithic and faunal evidence identify Uluzzo C as a central node of intensive and diverse technological production, while subsistence activities may have been primarily focused on late-stage carcass processing from selected skeletal elements.

6. Conclusions

The Mousterian faunal record from Uluzzo C highlights the complexity of depositional processes operating in cave and rock shelter contexts in southern Italy during the Late Pleistocene. The assemblages reflect a dynamic interplay between environmental conditions, human presence, and carnivore activity, resulting in stratified deposits characterised by palimpsest conditions rather than by single, discrete occupational events.
The taxonomic and ecological composition of the faunal remains points to a heterogeneous landscape combining open and wooded environments, consistent with a Mediterranean refugial setting. Such environmental diversity likely contributed to the recurrent use of the area over time, while also favouring the presence of multiple carnivore taxa, whose activities played a significant role in shaping the faunal assemblages. The alternating signatures of human and carnivore modification underscore the importance of considering non-anthropogenic contributions when interpreting Mousterian faunal records in similar settings. From a behavioural and spatial perspective, the evidence supports an interpretation of Uluzzo C as a location subject to intermittent and short-term human visits rather than prolonged or continuous occupation. This pattern is consistent with broader models of Middle Palaeolithic site use in ecologically rich but highly competitive landscapes, where caves and rock shelters functioned as repeatedly accessed places within wider mobility systems. Placed within a diachronic framework, the Mousterian deposits of Uluzzo C provide a critical point of reference for evaluating changes and continuities in site formation processes across the Middle to Upper Palaeolithic transition. Differences observed between the Mousterian and the overlying Uluzzian levels suggest that shifts in depositional dynamics and site use cannot be attributed solely to cultural change but must also be considered in relation to environmental conditions and the role of non-human agents.
More broadly, these results emphasise the interpretative value of zooarchaeological and taphonomic analyses for understanding the formation of archaeological deposits in Mediterranean contexts. Careful consideration of accumulation agents, palimpsest formation, and environmental proxies remains essential for constructing robust behavioural and palaeoenvironmental reconstructions, particularly in long and complex stratigraphic sequences, such as that of Uluzzo C. Ongoing excavations of Mousterian levels of the site will further contribute to refining these interpretations and to expanding the available dataset, allowing a more detailed assessment of depositional dynamics and environmental variability during the Middle Palaeolithic occupation of the site.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/quat9030037/s1, Figure S1: %NISP of each taxon from layers E, F and G of Uluzzo C; Figure S2: Percentage of thermal alterations from layers E (a) and G (b) of Uluzzo C; Figure S3: Box plots representing the different deamidation at Uluzzo C for both COL1α1 508–519 (m/z 1105.57) (left) and COL1α1 435–453 (m/z 1706.77) (right). Table S1: Fragmentation ratios from the three Mousterian layers of Uluzzo C. Teeth are excluded from N and %N of fractures on bones; Table S2: Fresh fractures in layers E, F and G of Uluzzo C by taxon and anatomical part; Table S3: Recognized taxon’s NISP (number of identified specimens) and MNE (minimum number of elements) values and percentages by unit for each element and combined anatomical region; Table S4: MNE (minimum number of elements), MAU (minimal animal units) and %MAU values for Bos/Bison, cervids and leporids of layer G from Uluzzo C, classified by anatomical part; Table S5: Spearman’s rank correlation analysis for Bos/Bison and cervids from layer G of Uluzzo C. Bivariate correlations are calculated between %MAU and bone density and the following indices: Meat, Marrow, Grease, FUI (Food Utility Index), CFUI (Corrected Food Utility Index), MGUI (Modified General Utility Index), UMI (Unsaturated Marrow Index). Spearman correlation coefficients and p-values are reported. Significant results are highlighted in bold; Table S6: Comparative dataset of Apulian faunal assemblages from Mousterian sites.

Author Contributions

Conceptualization, A.F., S.I.M.P., M.R. and G.T.; methodology, A.F., S.I.M.P., S.S., M.R. and G.T.; software, A.F., S.I.M.P., S.S., L.B. and G.T.; validation, A.F., S.I.M.P., S.S., G.S.N., O.B., F.B., A.M., M.R., G.T. and S.B.; formal analysis, A.F., S.I.M.P., S.S. and L.B.; investigation, A.F., S.I.M.P., S.S., L.B., A.M. and S.B.; resources, O.B., F.B., A.M. and S.B.; data curation, A.F., S.I.M.P., M.R. and G.T.; writing—original draft preparation, A.F., S.I.M.P., S.S., G.T. and S.B.; writing—review and editing, A.F., S.I.M.P., S.S., E.E.S., O.B., F.B., A.M., M.R., G.T. and S.B.; visualization, A.F., S.I.M.P., S.S., G.S.N., O.B., F.B., A.M., M.R., G.T. and S.B.; supervision, O.B., F.B., A.M., M.R., G.T. and S.B.; project administration, O.B., F.B. and S.B.; funding acquisition, O.B., F.B., A.M. and S.B. All authors have read and agreed to the published version of the manuscript.

Funding

The archaeological excavations at Uluzzo C were supported by the European Union—Next Generation EU PRIN 2022 “TRACE” (awarded to Stefano Benazzi and Adriana Moroni—Tracing early Homo sapiens in Italy) and by ERC Synergy Grant no.101118565 “LAST NEANDERTHALS” (awarded to Stefano Benazzi, Francesco Berna and Omry Barzilai).

Data Availability Statement

All raw data and MALDI-TOF-MS raw spectra can be found at Zenodo, doi: https://doi.org/10.5281/zenodo.19337295.

Acknowledgments

The authors are grateful to MiC that released the permits to excavate the site (Decreto del Direttore Generale rep. n. 259 del 18.3.2022), to the Soprintendenza Archeologia, Belle Arti e Paesaggio per le province di Brindisi, Lecce e Taranto as well as to the excavation and research team members. The authors thank Francesca Seghi and Francesca Borchi for having reported the presence of the materials. We are also grateful to the curators of the Museo di Storia Naturale di Firenze, Luca Bellucci and Stefano Dominici. During the preparation of this work, the authors used ChatGPT-5 and Claude to improve readability and language. After using this tool, the authors reviewed and edited the content as needed and assume full responsibility for the content of the publication.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Blasco, R.; Rosell, J.; Peris, J.F.; Arsuaga, J.L.; de Castro, J.M.B.; Carbonell, E. Environmental Availability, Behavioural Diversity and Diet: A Zooarchaeological Approach from the TD10-1 Sublevel of Gran Dolina (Sierra de Atapuerca, Burgos, Spain) and Bolomor Cave (Valencia, Spain). Quat. Sci. Rev. 2013, 70, 124–144. [Google Scholar] [CrossRef] [Scilit]
  2. Costamagno, S.; Beauval, C.; Lange-Badré, B.; Mann, A.; Maureille, B.; Vandermeersch, B. Homme Ou Carnivores? Protocole d’études d’ensembles Osseux Mixtes: L’exemple Du Gisement Moustérien Des Pradelles (Marillac-Le-Franc, Charente). Archaeofauna Int. J. Archaeozool. 2009, 14, 43–68. [Google Scholar]
  3. Hussain, S.T.; Weiss, M.; Nielsen, T.K. Being-with Other Predators: Cultural Negotiations of Neanderthal-Carnivore Relationships in Late Pleistocene Europe. J. Anthropol. Archaeol. 2022, 66, 101409. [Google Scholar] [CrossRef] [Scilit]
  4. Zilio, L.; Hammond, H.; Karampaglidis, T.; Sanchez-Romero, L.; Blasco, R.; Rivals, F.; Rufà, A.; Picin, A.; Chacon, M.G.; Demuro, M. Examining Neanderthal and Carnivore Occupations of Teixoneres Cave (Moià, Barcelona, Spain) Using Archaeostratigraphic and Intra-Site Spatial Analysis. Sci. Rep. 2021, 11, 4339. [Google Scholar] [CrossRef] [Scilit]
  5. Gómez-Olivencia, A.; Sala, N.; Núñez-Lahuerta, C.; Sanchis, A.; Arlegi, M.; Rios-Garaizar, J. First Data of Neandertal Bird and Carnivore Exploitation in the Cantabrian Region (Axlor; Barandiaran Excavations; Dima, Biscay, Northern Iberian Peninsula). Sci. Rep. 2018, 8, 10551. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Sanz-Royo, A.; Terlato, G.; Marín-Arroyo, A.B. Taphonomic Data from the Transitional Aurignacian of El Castillo Cave (Spain) Reveals the Role of Carnivores at the Aurignacian Delta Level. Quat. Sci. Adv. 2024, 13, 100147. [Google Scholar] [CrossRef] [Scilit]
  7. Douka, K.; Higham, T. The Chronological Factor in Understanding the Middle and Upper Paleolithic of Eurasia. Curr. Anthropol. 2017, 58, S480–S490. [Google Scholar] [CrossRef] [Scilit]
  8. Teyssandier, N. Us and Them: How to Reconcile Archaeological and Biological Data at the Middle-to-Upper Palaeolithic Transition in Europe? J. Paleolit. Archaeol. 2024, 7, 1. [Google Scholar] [CrossRef] [Scilit]
  9. Adler, D.S.; Bar-Oz, G.; Belfer-Cohen, A.; Bar-Yosef, O. Ahead of the Game: Middle and Upper Palaeolithic Hunting Behaviors in the Southern Caucasus. Curr. Anthropol. 2006, 47, 89–118. [Google Scholar] [CrossRef] [Scilit]
  10. Daujeard, C.; Vettese, D.; Britton, K.; Béarez, P.; Boulbes, N.; Crégut-Bonnoure, E.; Desclaux, E.; Lateur, N.; Pike-Tay, A.; Rivals, F.; et al. Neanderthal Selective Hunting of Reindeer? The Case Study of Abri Du Maras (South-Eastern France). Archaeol. Anthropol. Sci. 2019, 11, 985–1011. [Google Scholar] [CrossRef] [Scilit]
  11. Gaudzinski-Windheuser, S.; Niven, L. Hominin Subsistence Patterns During the Middle and Late Paleolithic in Northwestern Europe. In The Evolution of Hominin Diets: Integrating Approaches to the Study of Palaeolithic Subsistence; Hublin, J.-J., Richards, M.P., Eds.; Springer Netherlands: Dordrecht, The Netherlands, 2009; pp. 99–111. [Google Scholar]
  12. Grayson, D.K.; Delpech, F. Specialized Early Upper Palaeolithic Hunters in Southwestern France? J. Archaeol. Sci. 2002, 29, 1439–1449. [Google Scholar] [CrossRef] [Scilit]
  13. Livraghi, A.; Fanfarillo, G.; Dal Colle, M.; Romandini, M.; Peresani, M. Neanderthal Ecology and the Exploitation of Cervids and Bovids at the Onset of MIS4: A Study on De Nadale Cave, Italy. Quat. Int. 2021, 586, 24–41. [Google Scholar] [CrossRef] [Scilit]
  14. Marean, C.W.; Kim, S.Y. Mousterian Large-Mammal Remains from Kobeh Cave Behavioral Implications for Neanderthals and Early Modern Humans. Curr. Anthropol. 1998, 39, S79–S114. [Google Scholar] [CrossRef] [Scilit]
  15. Niven, L.; Steele, T.E.; Rendu, W.; Mallye, J.-B.; McPherron, S.P.; Soressi, M.; Jaubert, J.; Hublin, J.-J. Neandertal Mobility and Large-Game Hunting: The Exploitation of Reindeer during the Quina Mousterian at Chez-Pinaud Jonzac (Charente-Maritime, France). J. Hum. Evol. 2012, 63, 624–635. [Google Scholar] [CrossRef] [Scilit]
  16. Patou-Mathis, M. Neanderthal Subsistence Behaviours in Europe. Int. J. Osteoarchaeol. 2000, 10, 379–395. [Google Scholar] [CrossRef]
  17. Richards, M.P.; Trinkaus, E. Isotopic Evidence for the Diets of European Neanderthals and Early Modern Humans. Proc. Natl. Acad. Sci. USA 2009, 106, 16034–16039. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Speth, J.D.; Tchernov, E. The Middle Palaeolithic Occupations at Kebara Cave: A faunal perspective. In Kebara Cave, Mt. Carmel, Israel. The Middle and Upper Palaeolithic Archaeology; Peabody Museum of Archaeology and Ethnology, Harvard University: Cambridge, MA, USA, 2007; pp. 165–260. [Google Scholar]
  19. Stiner, M.C. Small Animal Exploitation and Its Relation to Hunting, Scavenging, and Gathering in the Italian Mousterian. Archaeol. Pap. Am. 1993, 4, 107–125. [Google Scholar] [CrossRef] [Scilit]
  20. Stiner, M.C. Honor Among Thieves. A Zoological Study of Neandertal Ecology; Princeton University Press: Princeton, NJ, USA, 1994. [Google Scholar]
  21. Stiner, M.C. An Unshakable Middle Paleolithic?: Trends versus Conservatism in the Predatory Niche and Their Social Ramifications. Curr. Anthropol. 2013, 54, S288–S304. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Terlato, G.; Livraghi, A.; Romandini, M.; Peresani, M. Large Bovids on the Neanderthal Menu: Exploitation of Bison priscus and Bos primigenius in Northeastern Italy. J. Archaeol. Sci. Rep. 2019, 25, 129–143. [Google Scholar] [CrossRef] [Scilit]
  23. Wißing, C.; Rougier, H.; Baumann, C.; Comeyne, A.; Crevecoeur, I.; Drucker, D.G.; Gaudzinski-Windheuser, S.; Germonpré, M.; Gómez-Olivencia, A.; Krause, J.; et al. Stable Isotopes Reveal Patterns of Diet and Mobility in the Last Neandertals and First Modern Humans in Europe. Sci. Rep. 2019, 9, 4433. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Blasco, R.; Rosell, J.; Smith, K.T.; Maul, L.C.; Sañudo, P.; Barkai, R.; Gopher, A. Tortoises as a Dietary Supplement: A View from the Middle Pleistocene Site of Qesem Cave, Israel. Quat. Sci. Rev. 2016, 133, 165–182. [Google Scholar] [CrossRef] [Scilit]
  25. Blasco, R.; Cochard, D.; Colonese, A.C.; Laroulandie, V.; Meier, J.; Morin, E.; Rufà, A.; Tassoni, L.; Thompson, J.C. Small Animal Use by Neanderthals. In Updating Neanderthals: Understanding Behavioural Complexity in the Late Middle Palaeolithic; Romagnoli, F., Rivals, F., Benazzi, S., Eds.; Academic Press: London, UK, 2022; pp. 123–143. [Google Scholar] [CrossRef] [Scilit]
  26. Boneta Jiménez, I.; Cardoso, J.L.; Pérez-García, A. The Turtles from the Middle Paleolithic Site of Gruta Nova Da Columbeira (Bombarral, Portugal): Update through an Archaeozoological Perspective. Anat. Rec. 2025, 308, 1677–1691. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Carvalho, M.; Pereira, T.; Manso, C. Rabbit Exploitation in the Middle Paleolithic at Gruta Nova Da Columbeira, Portugal. J. Archaeol. Sci. Rep. 2018, 21, 821–832. [Google Scholar] [CrossRef] [Scilit]
  28. Colonese, A.C.; Mannino, M.A.; Mayer, D.B.-Y.; Fa, D.A.; Finlayson, J.C.; Lubell, D.; Stiner, M.C. Marine Mollusc Exploitation in Mediterranean Prehistory: An Overview. Quat. Int. 2011, 239, 86–103. [Google Scholar] [CrossRef] [Scilit]
  29. Cortés-Sánchez, M.; Morales-Muñiz, A.; Simón-Vallejo, M.D.; Lozano-Francisco, M.C.; Vera-Peláez, J.L.; Finlayson, C.; Rodríguez-Vidal, J.; Delgado-Huertas, A.; Jiménez-Espejo, F.J.; Martínez-Ruiz, F.; et al. Earliest Known Use of Marine Resources by Neanderthals. PLoS ONE 2011, 6, e24026. [Google Scholar] [CrossRef] [Scilit]
  30. Finlayson, C.; Brown, K.; Blasco, R.; Rosell, J.; Negro, J.J.; Bortolotti, G.R.; Finlayson, G.; Sánchez Marco, A.; Giles Pacheco, F.; Rodríguez Vidal, J.; et al. Birds of a Feather: Neanderthal Exploitation of Raptors and Corvids. PLoS ONE 2012, 7, e45927. [Google Scholar] [CrossRef] [Scilit]
  31. Goffette, Q.; Rots, V.; Abrams, G.; Pirson, S.; Di Modica, K.; Bray, F.; Cnuts, D.; Bonjean, D.; Amos, L. Neanderthal Exploitation of Birds in North-Western Europe: Avian Remains from Scladina Cave (Belgium). Front. Environ. Archaeol. 2024, 3, 1441926. [Google Scholar] [CrossRef] [Scilit]
  32. Henry, A.G.; Brooks, A.S.; Piperno, D.R. Microfossils in Calculus Demonstrate Consumption of Plants and Cooked Foods in Neanderthal Diets (Shanidar III, Iraq; Spy I and II, Belgium). Proc. Natl. Acad. Sci. USA 2011, 108, 486–491. [Google Scholar] [CrossRef] [Scilit]
  33. Mata-González, M.; Starkovich, B.M.; Zeidi, M.; Conard, N.J. Evidence of Diverse Animal Exploitation during the Middle Paleolithic at Ghar-e Boof (Southern Zagros). Sci. Rep. 2023, 13, 19006. [Google Scholar] [CrossRef] [Scilit]
  34. Morin, E.; Bliege Bird, R.; Bird, D. Mass Procurement and Prey Rankings: Insights from the European Rabbit. Archaeol. Anthropol. Sci. 2020, 12, 262. [Google Scholar] [CrossRef] [Scilit]
  35. Pelletier, M.; Desclaux, E.; Brugal, J.-P.; Texier, P.-J. The Exploitation of Rabbits for Food and Pelts by Last Interglacial Neandertals. Quat. Sci. Rev. 2019, 224, 105972. [Google Scholar] [CrossRef] [Scilit]
  36. Peresani, M.; Fiore, I.; Gala, M.; Romandini, M.; Tagliacozzo, A. Late Neandertals and the Intentional Removal of Feathers as Evidenced from Bird Bone Taphonomy at Fumane Cave 44 Ky B.P., Italy. Proc. Natl. Acad. Sci. USA 2011, 108, 3888–3893. [Google Scholar] [CrossRef] [Scilit]
  37. Romandini, M.; Thun Hohenstein, U.; Fiore, I.; Tagliacozzo, A.; Perez, A.; Lubrano, V.; Terlato, G.; Peresani, M. Late Neandertals and the exploitation of small mammals in Northern Italy: Fortuity, necessity or hunting variability? Quaternaire. Rev. De L’association Française Pour L’étude Du Quat. 2018, 29, 61–67. [Google Scholar] [CrossRef] [Scilit]
  38. Stiner, M.C.; Munro, N.D.; Surovell, T.A. The Tortoise and the Hare: Small-Game Use, the Broad-Spectrum Revolution, and Paleolithic Demography. Curr. Anthropol. 2000, 41, 39–79. [Google Scholar] [CrossRef] [PubMed]
  39. Villa, P.; Soriano, S.; Pollarolo, L.; Smriglio, C.; Gaeta, M.; D’orazio, M.; Conforti, J.; Tozzi, C. Neandertals on the Beach: Use of Marine Resources at Grotta Dei Moscerini (Latium, Italy). PLoS ONE 2020, 15, e0226690. [Google Scholar] [CrossRef] [Scilit]
  40. Zilhão, J.; Angelucci, D.E.; Igreja, M.A.; Arnold, L.J.; Badal, E.; Callapez, P.; Cardoso, J.L.; d’Errico, F.; Daura, J.; Demuro, M.; et al. Last Interglacial Iberian Neandertals as Fisher-Hunter-Gatherers. Science 2020, 367, eaaz7943. [Google Scholar] [CrossRef] [Scilit]
  41. Douka, K.; Spinapolice, E.E. Neanderthal Shell Tool Production: Evidence from Middle Palaeolithic Italy and Greece. J. World Prehistory 2012, 25, 45–79. [Google Scholar] [CrossRef] [Scilit]
  42. Hardy, B.L.; Moncel, M.-H.; Daujeard, C.; Fernandes, P.; Béarez, P.; Desclaux, E.; Navarro, M.G.C.; Puaud, S.; Gallotti, R. Impossible Neanderthals? Making String, Throwing Projectiles and Catching Small Game during Marine Isotope Stage 4 (Abri Du Maras, France). Quat. Sci. Rev. 2013, 82, 23–40. [Google Scholar] [CrossRef] [Scilit]
  43. Nabais, M.; Zilhão, J. The Consumption of Tortoise among Last Interglacial Iberian Neanderthals. Quat. Sci. Rev. 2019, 217, 225–246. [Google Scholar] [CrossRef] [Scilit]
  44. Nabais, M.; Dupont, C.; Zilhão, J. The Exploitation of Crabs by Last Interglacial Iberian Neanderthals: The Evidence from Gruta Da Figueira Brava (Portugal). Front. Environ. Archaeol. 2023, 2, 1097815. [Google Scholar] [CrossRef] [Scilit]
  45. Sommer, R.S.; Zachos, F.E. Fossil Evidence and Phylogeography of Temperate Species: ‘Glacial Refugia’ and Post-glacial Recolonization. J. Biogeogr. 2009, 36, 2013–2020. [Google Scholar] [CrossRef] [Scilit]
  46. Ordonez, A.; Svenning, J.-C. Consistent Role of Quaternary Climate Change in Shaping Current Plant Functional Diversity Patterns across European Plant Orders. Sci. Rep. 2017, 7, 42988. [Google Scholar] [CrossRef] [Scilit]
  47. Morales-Barbero, J.; Martinez, P.A.; Ferrer-Castán, D.; Olalla-Tárraga, M.Á. Quaternary Refugia Are Associated with Higher Speciation Rates in Mammalian Faunas of the Western Palaearctic. Ecography 2018, 41, 607–621. [Google Scholar] [CrossRef] [Scilit]
  48. Benazzi, S.; Slon, V.; Talamo, S.; Negrino, F.; Peresani, M.; Bailey, S.E.; Sawyer, S.; Panetta, D.; Vicino, G.; Starnini, E.; et al. The Makers of the Protoaurignacian and Implications for Neandertal Extinction. Science 2015, 348, 793–796. [Google Scholar] [CrossRef] [Scilit]
  49. Boschin, F.; Columbu, A.; Spagnolo, V.; Crezzini, J.; Bahain, J.; FalguèRes, C.; Benazzi, S.; Boscato, P.; Ronchitelli, A.; Moroni, A.; et al. Human Occupation Continuity in Southern Italy towards the End of the Middle Palaeolithic: A Palaeoenvironmental Perspective from Apulia. J. Quat. Sci. 2022, 37, 204–216. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Higham, T.; Frouin, M.; Douka, K.; Ronchitelli, A.; Boscato, P.; Benazzi, S.; Crezzini, J.; Spagnolo, V.; McCarty, M.; Marciani, G.; et al. Chronometric Data and Stratigraphic Evidence Support Discontinuity between Neanderthals and Early Homo Sapiens in the Italian Peninsula. Nat. Commun. 2024, 15, 8016. [Google Scholar] [CrossRef] [Scilit]
  51. Riel-Salvatore, J. The Uluzzian and the Middle-Upper Paleolithic Transition in Southern Italy. Ph.D. Thesis, Arizona State University, Tempe, AZ, USA, 2007. [Google Scholar]
  52. Romandini, M.; Silvestrini, S.; Real, C.; Lugli, F.; Tassoni, L.; Carrera, L.; Badino, F.; Bortolini, E.; Marciani, G.; Delpiano, D. Late Neanderthal “Menu” from Northern to Southern Italy: Freshwater and Terrestrial Animal Resources. Quat. Sci. Rev. 2023, 315, 108233. [Google Scholar] [CrossRef] [Scilit]
  53. Boscato, P.; Crezzini, J. Il Deposito Musteriano Del Riparo l’Oscurusciuto (Ginosa–TA): La Fauna a Grandi Mammiferi Delle UUSS 1÷9. In Atti del 6 Convegno Nazionale di Archeozoologia; Associazione Italiana di Archeozoologia (AIAZ): Bolzano, Italy, 2012; pp. 25–32. [Google Scholar]
  54. Carrera, L.; Scarponi, D.; Martini, F.; Sarti, L.; Pavia, M. Mid-Late Pleistocene Neanderthal Landscapes in Southern Italy: Paleoecological Contributions of the Avian Assemblage from Grotta Del Cavallo, Apulia, Southern Italy. Palaeogeogr. Palaeoclimatol. Palaeoecol. 2021, 567, 110256. [Google Scholar] [CrossRef] [Scilit]
  55. Crezzini, J.; Boscato, P.; Ronchitelli, A.; Boschin, F. A Peculiar Exploitation of Ungulates at Grotta Di Santa Croce: Bone Grease Rendering and Nutritional Patterns among Neanderthals in Southern Italy. Hist. Biol. 2024, 36, 2133–2145. [Google Scholar] [CrossRef] [Scilit]
  56. Borzatti von Löwenstern, E. La Grotta-Riparo Di Uluzzo C. Riv. Di Sci. Preist. 1965, 20, 1–31. [Google Scholar]
  57. Borzatti von Löwenstern, E. Alcuni Aspetti Del Musteriano Nel Salento: La Grotta-Riparo Di Torre Dell’Alto e La Grotta Di Uluzzo C. Scavi 1965 e 1966. Riv. Di Sci. Preist. 1966, 21, 203–287. [Google Scholar]
  58. Borzatti von Löwenstern, E.; Magaldi, D. Risultati Conclusivi Dello Studio Paletnologico e Sedimentologico Della Grotta Di Uluzzo C (Nardò, Lecce). Riv. Di Sci. Preist. 1969, 24, 15–64. [Google Scholar]
  59. Fiorini, A.; Curci, A.; Spinapolice, E.E.; Benazzi, S. Grotta Di Uluzzo C (Nardò-Lecce). Risultati Preliminari, Strumenti e Metodi Dell’indagine Archeologica. FOLDR 2019, 1–18. [Google Scholar]
  60. Ochando, J.; Magri, D.; Carrión, J.S.; Giaccio, B.; Zanchetta, G.; Vazzana, A.; Barzilai, O.; Berna, F.; Neretino, G.S.; Marciani, G.; et al. From Neanderthals to Homo Sapiens: New Palaeoecological and Tephrocronological Data from the MIS3 Layers of Grotta-Riparo Di Uluzzo C (Apulia, Southern Italy). Quat. Sci. Rev. 2026, 376, 109830. [Google Scholar] [CrossRef] [Scilit]
  61. Seghi, F.; Sorrentino, R.; Bailey, S.E.; Piccirilli, E.; Vazzana, A.; Bortolini, E.; Higgins, O.A.; Marciani, G.; Orlando, M.A.; Spinapolice, E.E.; et al. Morphological and Morphometric Study of the Hominin Dental Casts from Grotta-Riparo Di Uluzzo C (Apulia, Southern Italy). Am. J. Biol. Anthropol. 2024, 185, e24998. [Google Scholar] [CrossRef] [Scilit]
  62. Silvestrini, S.; Lugli, F.; Romandini, M.; Real, C.; Sommella, E.; Salviati, E.; Arrighi, S.; Bortolini, E.; Figus, C.; Higgins, O.A. Integrating ZooMS and Zooarchaeology: New Data from the Uluzzian Levels of Uluzzo C Rock Shelter, Roccia San Sebastiano Cave and Riparo Del Broion. PLoS ONE 2022, 17, e0275614. [Google Scholar] [CrossRef] [Scilit]
  63. Silvestrini, S.; Romandini, M.; Marciani, G.; Arrighi, S.; Carrera, L.; Fiorini, A.; López-García, J.M.; Lugli, F.; Ranaldo, F.; Slon, V.; et al. Integrated Multidisciplinary Ecological Analysis from the Uluzzian Settlement at the Uluzzo C Rock Shelter, South-eastern Italy. J. Quat. Sci. 2022, 37, 235–256. [Google Scholar] [CrossRef] [Scilit]
  64. Silvestrini, S.; Real, C.; Lugli, F.; Delpiano, D.; Harvati, K.; Collina, C.; Peresani, M.; Spinapolice, E.E.; Romandini, M.; Benazzi, S. Hunting Game: New Data on the Subsistence Strategies during the Uluzzian in Italy. J. Archaeol. Sci. Rep. 2024, 57, 104575. [Google Scholar] [CrossRef] [Scilit]
  65. Spinapolice, E.E.; Zerboni, A.; Meyer, M.C.; Talamo, S.; Mariani, G.S.; Gliganic, L.A.; Buti, L.; Fusco, M.; Maiorano, M.P.; Silvestrini, S.; et al. Back to Uluzzo—Archaeological, Palaeoenvironmental and Chronological Context of the Mid–Upper Palaeolithic Sequence at Uluzzo C Rock Shelter (Apulia, Southern Italy). J. Quat. Sci. 2022, 37, 217–234. [Google Scholar] [CrossRef] [Scilit]
  66. Cosma, C. Attività Del Circolo Speleologico “Pasquale de Lorentiis” Di Lecce: Le Grotte Di “U Luzzu” in Agro Di Nardò. Quat. Stor. Nat. E Cult. Del Quat. 1960, 5, 363–364. [Google Scholar]
  67. Zanchetta, G.; Bini, M.; Giaccio, B.; Mele, D. I Livelli Vulcanoclastici: Analisi Chimica e Considerazioni Deposizionali. In Il Musteriano di Grotta del Cavallo nel Salento (Scavi 1986–2005). Cultura e ambienti; Museo e Istituto Fiorentino di Preistoria Paolo Graziosi: Florence, Italy, 2020; pp. 53–64. [Google Scholar]
  68. Sarti, L.; Martini, F. (Eds.) Il Musteriano Di Grotta Del Cavallo Nel Salento (Scavi 1986-2005): Culture e Ambienti; Museo e Istituto Fiorentino di Preistoria “Paolo Graziosi”: Florence, Italy, 2020. [Google Scholar]
  69. Zanchetta, G.; Giaccio, B.; Bini, M.; Sarti, L. Tephrostratigraphy of Grotta del Cavallo, Southern Italy: Insights on the chronology of Middle to Upper Palaeolithic transition in the Mediterranean. Quat. Sci. Rev. 2018, 182, 65–77. [Google Scholar] [CrossRef] [Scilit]
  70. Mastronuzzi, G.; Sansò, P. Pleistocene Sea-Level Changes, Sapping Processes and Development of Valley Networks in the Apulia Region (Southern Italy). Geomorphology 2002, 46, 19–34. [Google Scholar] [CrossRef] [Scilit]
  71. Mastronuzzi, G.; Quinif, Y.; Sansò, P.; Selleri, G. Middle-Late Pleistocene Polycyclic Evolution of a Stable Coastal Area (Southern Apulia, Italy). Geomorphology 2007, 86, 393–408. [Google Scholar] [CrossRef] [Scilit]
  72. Barone, R. Anatomia Comparata Dei Mammiferi Domestici; Edagricole: Milan, Italy, 1980. [Google Scholar]
  73. Cohen, A.; Serjeantson, D. A Manual for the Identification of Bird Bones from Archaeological Sites; Archetype Publications: London, UK, 1996. [Google Scholar]
  74. Pales, L.; Lambert, C. Atlas Ostéologique Pour Servir à l’identification Des Mammifères Du Quaternaire; Éditions du Centre National de la Recherche Scientifique: Paris, France, 1971; pp. 1–77. [Google Scholar]
  75. Schmid, E. Atlas of Animal Bones/Knochenatlas; Elsevier: Amsterdam, The Netherlands; London, UK; New York, NY, USA, 1972. [Google Scholar]
  76. Binford, L.R. Butchering, Sharing, and the Archaeological Record. J. Anthropol. Archaeol. 1984, 3, 235–257. [Google Scholar] [CrossRef] [Scilit]
  77. Brain, C.K. The Hunters or the Hunted?: An Introduction to African Cave Taphonomy; University of Chicago Press: Chicago, IL, USA, 1983. [Google Scholar]
  78. Lyman, R.L. Vertebrate Taphonomy; Cambridge University Press: Cambridge, UK, 1994. [Google Scholar]
  79. Romandini, M. Analisi Archeozoologica, Tafonomica, Paleontologica e Spaziale Dei Livelli Uluzziani e Tardo-Musteriani Della Grotta Di Fumane (VR). Variazioni e Continuità Strategicocomportamentali Umane in Italia Nord Orientale: I Casi Di Grotta Del Col Della Stria (VI) e Grotta Del Rio Secco (PN). Ph.D. Thesis, Università degli Studi di Ferrara, Ferrara, Italy, 2012. [Google Scholar]
  80. Marean, C.W.; Abe, Y.; Nilssen, P.J.; Stone, E.C. Estimating the Minimum Number of Skeletal Elements (MNE) in Zooarchaeology: A Review and a New Image-Analysis GIS Approach. Am. Antiq. 2001, 66, 333–348. [Google Scholar] [CrossRef] [Scilit]
  81. Silver, I.A. The Ageing of Domestic Animals. In Science in Archaeology; Brothwell, D., Higgs, E., Eds.; Thames & Hudson: London, UK, 1969. [Google Scholar]
  82. Azorit, C. Guía Para La Determinación de La Edad Del Ciervo Ibérico (Cervus Elaphus Hispanicus) a Través de Su Dentición: Revisión Metodológica y Técnicas de Elección. An. Real Acad. Cienc. Vet. Andal. Orient. 2011, 24, 235–264. [Google Scholar]
  83. Mariezkurrena, K. Contribución al Conocimiento Del Desarrollo de La Dentición y El Esqueleto Postcraneal de Cervus elaphus. Munibe 1983, 35, 149–202. [Google Scholar]
  84. Marín, J.; Saladié, P.; Azorit, C.; Rodríguez-Hidalgo, A. Identification of Age at Death in Red Deer (Cervus elaphus) through the Upper Dentition: Eruption Pattern, Wear Stage and Crown Heights. J. Archaeol. Sci. 2024, 163, 105934. [Google Scholar] [CrossRef] [Scilit]
  85. Tomé, C.; Vigne, J.-D. Roe Deer (Capreolus capreolus) Age at Death Estimates: New Methods and Modern Reference Data for Tooth Eruption and Wear, and for Epiphyseal Fusion. Archaeofauna Int. J. Archaeozool. 2003, 12, 157–173. [Google Scholar] [CrossRef] [Scilit]
  86. Couturier, M.A.J. Le Bouquetin des Alpes; Arthaud: Grenoble, France, 1962. [Google Scholar]
  87. Habermehl, K.-H. Die Altersbestimmung Bei Haustieren, Pelztieren Und Beim Jagdbaren Wild; Parey: Berlin/Heidelberg, Germany, 1961; pp. 146–153. [Google Scholar]
  88. Habermehl, K. Die Altersbeurteilung Beim Weiblichen Steinwild (Capra ibex ibex L.) Anhand Der Skelettentwicklung. Anat. Histol. Embryol. 1992, 21, 193–198. [Google Scholar] [CrossRef] [Scilit]
  89. Pflieger, R. Le Chamois: Son Identification et Sa Vie; Gerfaut Club Princesse: Chartres, France, 1982. [Google Scholar]
  90. Fernandez, P.; Legendre, S. Mortality Curves for Horses from the Middle Palaeolithic Site of Bau de l’Aubesier (Vaucluse, France): Methodological, Palaeo-Ethnological, and Palaeo-Ecological Approaches. J. Archaeol. Sci. 2003, 30, 1577–1598. [Google Scholar] [CrossRef] [Scilit]
  91. Broekhuizen, S.; Maaskamp, F. Annual Production of Young in European Hares (Lepus europaeus) in the Netherlands. J. Zool. 1981, 193, 499–516. [Google Scholar] [CrossRef] [Scilit]
  92. Gardeisen, A.; Valenzuela-Lamas, S. À Propos de La Présence de Lapins En Contexte Gallo-Romain à Lattara (Lattes, Hérault, France). In Petits Animaux et Sociétés Humaines, XXIVèmes Rencontres Internationales D’archéologie et D’histoire d’Antibes; Editions APDCA: Antibes, France, 2004; pp. 235–354. [Google Scholar]
  93. Jones, E.L. Prey Choice, Mass Collecting, and the Wild European Rabbit (Oryctolagus cuniculus). J. Anthropol. Archaeol. 2006, 25, 275–289. [Google Scholar] [CrossRef] [Scilit]
  94. Discamps, E.; Costamagno, S. Improving Mortality Profile Analysis in Zooarchaeology: A Revised Zoning for Ternary Diagrams. J. Archaeol. Sci. 2015, 58, 62–76. [Google Scholar] [CrossRef] [Scilit]
  95. Stiner, M.C. The Use of Mortality Patterns in Archaeological Studies of Hominid Predatory Adaptations. J. Anthropol. Archaeol. 1990, 9, 305–351. [Google Scholar] [CrossRef] [Scilit]
  96. Binford, L.R. Dimensional Analysis of Behavior and Site Structure: Learning from an Eskimo Hunting Stand. Am. Antiq. 1978, 43, 330–361. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  97. Metcalfe, D.; Jones, K.T. A Reconsideration of Animal Body-Part Utility Indices. Am. Antiq. 1988, 53, 486–504. [Google Scholar] [CrossRef] [Scilit]
  98. Morin, E. Fat Composition and Nunamiut Decision-Making: A New Look at the Marrow and Bone Grease Indices. J. Archaeol. Sci. 2007, 34, 69–82. [Google Scholar] [CrossRef] [Scilit]
  99. Hammer, Ø.; Harper, D.A. Past: Paleontological Statistics Software Package for Educaton and Data Anlysis. Palaeontol. Electron. 2001, 4, 1. [Google Scholar]
  100. Simpson, E.H. Measurement of Diversity. Nature 1949, 163, 688. [Google Scholar] [CrossRef] [Scilit]
  101. Magurran, A.E. Ecological Diversity and Its Measurement; Princeton University Press: Princeton, NJ, USA, 2013. [Google Scholar]
  102. Binford, L.R. Bones: Ancient Men and Modern Myths; Academic Press: New York, NY, USA, 1981. [Google Scholar]
  103. Lyman, R.L. Quantitative Paleozoology; Cambridge University Press: Cambridge, UK, 2008. [Google Scholar]
  104. Potts, R.; Shipman, P. Cutmarks Made by Stone Tools on Bones from Olduvai Gorge, Tanzania. Nature 1981, 291, 577–580. [Google Scholar] [CrossRef] [Scilit]
  105. Shipman, P. Life History of a Fossil: An Introduction to Taphonomy and Paleoecology; Harvard University Press: Cambridge, MA, USA, 1981. [Google Scholar]
  106. Shipman, P.; Rose, J. Early Hominid Hunting, Butchering, and Carcass-Processing Behaviors: Approaches to the Fossil Record. J. Anthropol. Archaeol. 1983, 2, 57–98. [Google Scholar] [CrossRef] [Scilit]
  107. Costamagno, S.; David, F. Comparaison Des Pratiques Bouchères et Culinaires de Différents Groupes Sibériens Vivant de La Renniculture. Archaeofauna Int. J. Archaeozool. 2009, 18, 9–25. Available online: https://hal.science/hal-00431301v1 (accessed on 22 January 2024).
  108. Fisher, J.W. Bone Surface Modifications in Zooarchaeology. J. Archaeol. Method Theory 1995, 2, 7–68. [Google Scholar] [CrossRef] [Scilit]
  109. Galán, A.B.; Domínguez-Rodrigo, M. An Experimental Study of the Anatomical Distribution of Cut Marks Created by Filleting and Disarticulation on Long Bone Ends. Archaeometry 2013, 55, 1132–1149. [Google Scholar] [CrossRef] [Scilit]
  110. Nilssen, P.J. An Actualistic Butchery Study in South Africa and Its Implications for Reconstructing Hominid Strategies of Carcass Acquisition and Butchery in the Upper Pleistocene and Plio-Pleistocene. Ph.D. Thesis, University of Cape Town, Western Cape, South Africa, 2000. [Google Scholar]
  111. Soulier, M.-C. L’exploitation Alimentaire et Technique Du Gibier Au Début Du Paléolithique Supérieur Aux Abeilles (Haute-Garonne, France). PALEO. Rev. D’archéologie Préhistorique 2014, 25, 287–307. [Google Scholar] [CrossRef] [Scilit]
  112. Soulier, M.-C.; Costamagno, S. Let the Cutmarks Speak! Experimental Butchery to Reconstruct Carcass Processing. J. Archaeol. Sci. Rep. 2017, 11, 782–802. [Google Scholar] [CrossRef] [Scilit]
  113. Soulier, M.-C.; Morin, E. Cutmark Data and Their Implications for the Planning Depth of Late Pleistocene Societies. J. Hum. Evol. 2016, 97, 37–57. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  114. Villa, P.; Mahieu, E. Breakage Patterns of Human Long Bones. J. Hum. Evol. 1991, 21, 27–48. [Google Scholar] [CrossRef] [Scilit]
  115. Bunn, H.T. Archaeological Evidence for Meat-Eating by Plio-Pleistocene Hominids from Koobi Fora and Olduvai Gorge. Nature 1981, 291, 574–577. [Google Scholar] [CrossRef] [Scilit]
  116. Blumenschine, R.J.; Selvaggio, M.M. Percussion Marks on Bone Surfaces as a New Diagnostic of Hominid Behaviour. Nature 1988, 333, 763–765. [Google Scholar] [CrossRef] [Scilit]
  117. Capaldo, S.D.; Blumenschine, R.J. A Quantitative Diagnosis of Notches Made by Hammerstone Percussion and Carnivore Gnawing on Bovid Long Bones. Am. Antiq. 1994, 59, 724–748. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  118. Galán, A.B.; Rodríguez, M.; De Juana, S.; Domínguez-Rodrigo, M. A New Experimental Study on Percussion Marks and Notches and Their Bearing on the Interpretation of Hammerstone-Broken Faunal Assemblages. J. Archaeol. Sci. 2009, 36, 776–784. [Google Scholar] [CrossRef] [Scilit]
  119. Pickering, T.R.; Egeland, C.P. Experimental Patterns of Hammerstone Percussion Damage on Bones: Implications for Inferences of Carcass Processing by Humans. J. Archaeol. Sci. 2006, 33, 459–469. [Google Scholar] [CrossRef] [Scilit]
  120. Pickering, T.R.; Domínguez-Rodrigo, M.; Heaton, J.L.; Yravedra, J.; Barba, R.; Bunn, H.T.; Musiba, C.; Baquedano, E.; Diez-Martín, F.; Mabulla, A.; et al. Taphonomy of Ungulate Ribs and the Consumption of Meat and Bone by 1.2-Million-Year-Old Hominins at Olduvai Gorge, Tanzania. J. Archaeol. Sci. 2013, 40, 1295–1309. [Google Scholar] [CrossRef] [Scilit]
  121. Vettese, D.; Blasco, R.; Cáceres, I.; Gaudzinski-Windheuser, S.; Moncel, M.-H.; Hohenstein, U.T.; Daujeard, C. Towards an Understanding of Hominin Marrow Extraction Strategies: A Proposal for a Percussion Mark Terminology. Archaeol. Anthropol. Sci. 2020, 12, 48. [Google Scholar] [CrossRef] [Scilit]
  122. Vettese, D.; Stavrova, T.; Borel, A.; Marín, J.; Moncel, M.-H.; Arzarello, M.; Daujeard, C. A Way to Break Bones? The Weight of Intuitiveness. PLoS ONE 2021, 16, e0259136. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  123. Coil, R.; Yezzi-Woodley, K.; Tappen, M. Comparisons of Impact Flakes Derived from Hyena and Hammerstone Long Bone Breakage. J. Archaeol. Sci. 2020, 120, 105167. [Google Scholar] [CrossRef] [Scilit]
  124. Stiner, M.C.; Kuhn, S.L.; Weiner, S.; Bar-Yosef, O. Differential Burning, Recrystallization, and Fragmentation of Archaeological Bone. J. Archaeol. Sci. 1995, 22, 223–237. [Google Scholar] [CrossRef] [Scilit]
  125. Blumenschine, R.J. Percussion Marks, Tooth Marks, and Experimental Determinations of the Timing of Hominid and Carnivore Access to Long Bones at FLK Zinjanthropus, Olduvai Gorge, Tanzania. J. Hum. Evol. 1995, 29, 21–51. [Google Scholar] [CrossRef] [Scilit]
  126. Domínguez-Rodrigo, M.; Piqueras, A. The Use of Tooth Pits to Identify Carnivore Taxa in Tooth-Marked Archaeofaunas and Their Relevance to Reconstruct Hominid Carcass Processing Behaviours. J. Archaeol. Sci. 2003, 30, 1385–1391. [Google Scholar] [CrossRef] [Scilit]
  127. Domínguez-Rodrigo, M.; Barba, R. New Estimates of Tooth Mark and Percussion Mark Frequencies at the FLK Zinj Site: The Carnivore-Hominid-Carnivore Hypothesis Falsified. J. Hum. Evol. 2006, 50, 170–194. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  128. Fernández-Jalvo, Y.; Andrews, P. Atlas of Taphonomic Identifications: 1001+ Images of Fossil and Recent Mammal Bone Modification; Springer: Berlin/Heidelberg, Germany, 2016. [Google Scholar]
  129. Behrensmeyer, A.K. Taphonomic and Ecologic Information from Bone Weathering. Paleobiology 1978, 4, 150–162. [Google Scholar] [CrossRef] [Scilit]
  130. Blasco, R.; Rosell, J.; Peris, J.F.; Cáceres, I.; Vergès, J.M. A New Element of Trampling: An Experimental Application on the Level XII Faunal Record of Bolomor Cave (Valencia, Spain). J. Archaeol. Sci. 2008, 35, 1605–1618. [Google Scholar] [CrossRef] [Scilit]
  131. Domínguez-Rodrigo, M.; De Juana, S.; Galan, A.B.; Rodríguez, M. A New Protocol to Differentiate Trampling Marks from Butchery Cut Marks. J. Archaeol. Sci. 2009, 36, 2643–2654. [Google Scholar] [CrossRef] [Scilit]
  132. Buckley, M.; Collins, M.; Thomas-Oates, J.; Wilson, J.C. Species Identification by Analysis of Bone Collagen Using Matrix-assisted Laser Desorption/Ionisation Time-of-flight Mass Spectrometry. Rapid Commun. Mass Spectrom. 2009, 23, 3843–3854. [Google Scholar] [CrossRef] [Scilit]
  133. Strohalm, M.; Kavan, D.; Novák, P.; Volný, M.; Havlíček, V. mMass 3: A Cross-Platform Software Environment for Precise Analysis of Mass Spectrometric Data. Anal. Chem. 2010, 82, 4648–4651. [Google Scholar] [CrossRef] [Scilit]
  134. Wang, N.; Brown, S.; Ditchfield, P.; Hebestreit, S.; Kozilikin, M.; Luu, S.; Wedage, O.; Grimaldi, S.; Chazan, M.; Horowitz Kolska, L.; et al. Testing the Efficacy and Comparability of ZooMS Protocols on Archaeological Bone. J. Proteom. 2021, 233, 104078. [Google Scholar] [CrossRef] [Scilit]
  135. Welker, F.; Hajdinjak, M.; Talamo, S.; Jaouen, K.; Dannemann, M.; David, F.; Julien, M.; Meyer, M.; Kelso, J.; Barnes, I.; et al. Palaeoproteomic Evidence Identifies Archaic Hominins Associated with the Châtelperronian at the Grotte Du Renne. Proc. Natl. Acad. Sci. USA 2016, 113, 11162–11167. [Google Scholar] [CrossRef] [Scilit]
  136. Jensen, T.Z.T.; Sjöström, A.; Fischer, A.; Rosengren, E.; Lanigan, L.T.; Bennike, O.; Richter, K.K.; Gron, K.J.; Mackie, M.; Mortensen, M.F.; et al. An Integrated Analysis of Maglemose Bone Points Reframes the Early Mesolithic of Southern Scandinavia. Sci. Rep. 2020, 10, 17244. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  137. Janzen, A.; Richter, K.K.; Mwebi, O.; Brown, S.; Onduso, V.; Gatwiri, F.; Ndiema, E.; Katongo, M.; Goldstein, S.T.; Douka, K.; et al. Distinguishing African Bovids Using Zooarchaeology by Mass Spectrometry (ZooMS): New Peptide Markers and Insights into Iron Age Economies in Zambia. PLoS ONE 2021, 16, e0251061. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  138. Xia, H.; Zhang, D.; Wang, J.; Fagernäs, Z.; Li, T.; Li, Y.; Yao, J.; Lin, D.; Troché, G.; Smith, G.M.; et al. Middle and Late Pleistocene Denisovan Subsistence at Baishiya Karst Cave. Nature 2024, 632, 108–113. [Google Scholar] [CrossRef] [Scilit]
  139. Schroeter, E.R.; Cleland, T.P. Glutamine Deamidation: An Indicator of Antiquity, or Preservational Quality? Rapid Commun. Mass Spectrom. 2016, 30, 251–255. [Google Scholar] [CrossRef] [Scilit]
  140. Wilson, J.; Van Doorn, N.L.; Collins, M.J. Assessing the Extent of Bone Degradation Using Glutamine Deamidation in Collagen. Anal. Chem. 2012, 84, 9041–9048. [Google Scholar] [CrossRef] [Scilit]
  141. Conti, N.; Petronio, C.; Salari, L. The Late Pleistocene Equids from “Tana Delle Iene” (Ceglie Messapica, Brindisi, Southern Italy). Bull. Della Soc. Paleontol. Ital. 2010, 49, 227–236. [Google Scholar]
  142. Pandolfi, L.; Petronio, C.; Salari, L. Catastrophic Death Assemblages from the Late Pleistocene of Italy: The Case of Avetrana Karst Filling (Taranto, Southern Italy). Riv. Ital. Di Paleontol. E Stratigr. 2013, 119, 109–124. [Google Scholar] [CrossRef] [Scilit]
  143. Boitani, L.; Lovari, S.; Taglianti, A.V. Mammalia III; Calderini: Bologna, Italy, 2003. [Google Scholar]
  144. Riel-Salvatore, J.; Negrino, F. Early Upper Paleolithic Population Dynamics and Raw Material Procurement Patterns in Italy. In The Mediterranean from 50000 to 25000 BP: Turning Points and New Directions; Oxbow Books: Oxford, UK, 2009; pp. 211–230. [Google Scholar]
  145. Columbu, A.; Chiarini, V.; Spötl, C.; Benazzi, S.; Hellstrom, J.; Cheng, H.; De Waele, J. Speleothem Record Attests to Stable Environmental Conditions during Neanderthal–Modern Human Turnover in Southern Italy. Nat. Ecol. Evol. 2020, 4, 1188–1195. [Google Scholar] [CrossRef] [Scilit]
  146. Di Stefano, G.; Petronio, C.; Salari, L. Review of the First Occurrences of Some Selected Late Pleistocene Italian Mammals. Boll. Mus. Civ. Stor. Nat. Verona 2023, 47, 49–68. [Google Scholar]
  147. Petronio, C.; Di Stefano, G.; Kotsakis, T.; Salari, L.; Marra, F.; Jicha, B.R. Biochronological Framework for the Late Galerian and Early-Middle Aurelian Mammal Ages of Peninsular Italy. Geobios 2019, 53, 35–50. [Google Scholar] [CrossRef] [Scilit]
  148. Petronio, C.; Di Canzio, E.; Salari, L. The Late Pleistocene and Holocene Mammals in Italy: New Biochronological and Paleoenvironmental Data. Palaeontogr. Abt. A 2007, 279, 147–157. [Google Scholar] [CrossRef] [Scilit]
  149. Pandolfi, L.; Bartolini-Lucenti, S.; Cirilli, O.; Bukhsianidze, M.; Lordkipanidze, D.; Rook, L. Paleoecology, Biochronology, and Paleobiogeography of Eurasian Rhinocerotidae during the Early Pleistocene: The Contribution of the Fossil Material from Dmanisi (Georgia, Southern Caucasus). J. Hum. Evol. 2021, 156, 103013. [Google Scholar] [CrossRef] [Scilit]
  150. Saarinen, J.; Eronen, J.; Fortelius, M.; Seppä, H.; Lister, A.M.L.H. Patterns of Diet and Body Mass of Large Ungulates from the Pleistocene of Western Europe, and Their Relation to Vegetation. Palaeontol. Electron. 2016, 19.3.32A, 1–58. [Google Scholar] [CrossRef] [Scilit]
  151. Burkanova, E.M.; Billia, E.M.E.; Persico, D. Stephanorhinus kirchbergensis (Jäger, 1839) (Mammalia, Rhinocerotidae) from the Po Valley (Lombardia, Northern Italy): Possible Diet/Nutrition and Living Conditions. Quat. Int. 2020, 554, 164–169. [Google Scholar] [CrossRef] [Scilit]
  152. Pandolfi, L. Reassessing the Phylogeny of Quaternary Eurasian Rhinocerotidae. J. Quat. Sci. 2023, 38, 291–294. [Google Scholar] [CrossRef] [Scilit]
  153. Boscato, P. Ambienti Ed Economia Nel Paleolitico Medio Della Puglia: Lo Studio Delle Faune. Preist. E Protostoria Della Puglia (Studi Preist. E Protostoria) 2017, 4, 119–124. [Google Scholar]
  154. Dalla Valle, C. I Micromammiferi Dei Livelli Musteriani e Romanelliani Della Grotta Del Cavallo (Lecce). Ph.D. Thesis, Università Cà Foscari di Venezia, Venice, Italy, 2008. [Google Scholar]
  155. Sarti, L.; Boscato, P.; Martini, F.; Spagnoletti, P. Il Musteriano Di Grotta Del Cavallo-Strati H e I: Studio Preliminare. Riv. Di Sci. Preist. 2002, 52, 21–109. [Google Scholar]
  156. Boscato, P.; Gambassini, P.; Ranaldo, F.; Ronchitelli, A. Management of Paleoenvironmental Resources and Exploitation of Raw Materials at the Middle Paleolithic Site of Oscurusciuto (Ginosa, Southern Italy): Units 1 and 4. In Neanderthal Lifeways, Subsistence and Technology; Vertebrate Paleobiology and Paleoanthropology; Conard, N.J., Richter, J., Eds.; Springer Netherlands: Dordrecht, The Netherlands, 2011; Volume 19, pp. 87–96. [Google Scholar] [CrossRef] [Scilit]
  157. Spagnolo, V.; Marciani, G.; Aureli, D.; Berna, F.; Boscato, P.; Ranaldo, F.; Ronchitelli, A. Between Hearths and Volcanic Ash: The SU 13 Palimpsest of the Oscurusciuto Rock Shelter (Ginosa–Southern Italy): Analytical and Interpretative Questions. Quat. Int. 2016, 417, 105–121. [Google Scholar] [CrossRef] [Scilit]
  158. Crezzini, J.; Modi, A.; Cannariato, C.; Caramelli, D.; Ronchitelli, A.; Boscato, P.; Moroni, A.; Boschin, F. Neanderthal Had a “Crush” on Fats. Macronutrient Estimation in Middle Paleolithic (Late Mousterian) Hunter-Gatherers of Southern Italy. Front. Environ. Archaeol. 2025, 4, 1558698. [Google Scholar] [CrossRef] [Scilit]
  159. Mecozzi, B. Le Faune a Mammiferi Del Pleistocene Medio-Superiore Della Puglia: Biocronologia, Paleoecologia, Paleobiogeografia. Ph.D. Thesis, Sapienza Università di Roma, Rome, Italy, 2019. [Google Scholar]
  160. Mecozzi, B.; Bona, F.; Conti, J.; Lembo, G.; Mariani, G.S.; Mazzini, I.; Muttillo, B.; Pieruccini, P.; Sardella, R. Large Mammal Faunas and Ecosystem Dynamics during the Late Middle to Early Late Pleistocene at Grotta Romanelli (Southern Italy). Quat. Sci. Adv. 2024, 16, 100237. [Google Scholar] [CrossRef] [Scilit]
  161. Pandolfi, L.; Tagliacozzo, A. Earliest Occurrence of Woolly Rhino (Coelodonta antiquitatis) in Italy (Late Pleistocene, Grotta Romanelli Site). Riv. Ital. Paleontol. E Stratigr. 2013, 119, 125–129. [Google Scholar]
  162. Sardella, R.; Bertè, D.; Iurino, D.A.; Cherin, M.; Tagliacozzo, A. The Wolf from Grotta Romanelli (Apulia, Italy) and Its Implications in the Evolutionary History of Canis lupus in the Late Pleistocene of Southern Italy. Quat. Int. 2014, 328, 179–195. [Google Scholar] [CrossRef] [Scilit]
  163. Sardella, R.; Mazzini, I.; Giustini, F.; Mecozzi, B.; Brilli, M.; Iurino, D.A.; Lembo, G.; Muttillo, B.; Massussi, M.; Sigari, D. Grotta Romanelli (Southern Italy, Apulia): Legacies and Issues in Excavating a Key Site for the Pleistocene of the Mediterranean. Riv. Ital. Paleontol. E Stratigr. 2018, 124, 247–264. [Google Scholar] [CrossRef]
  164. Petronio, C.; Bellardini, F.; Arzarello, M.; Bedetti, C.; Bellucci, L.; Cipullo, A.; Di Stefano, G.; Pandolfi, L.; Pavia, M.; Petrucci, M. The Deposit of the Late Pleistocene from Avetrana (Taranto, Southern Italy): Biochronology and Palaeoecology. Il Quat. 2008, 21, 409–422. [Google Scholar]
  165. Salari, L.; Petronio, C.; Kotsakis, T.; Di Stefano, G.; Grossi, F.; Maiorino, L.; Pandolfi, L.; Federico Rolfo, M.; Daniela Ruiu, F.; Sansalone, G. Reassessing the Faunal Assemblages of the Late Pleistocene Stratified Karst Filling from Avetrana (Apulia, Southern Italy): The Bed 8, Palaeoenvironment and Biochronology. Alp. Mediterr. Quat. 2019, 32, 101–115. [Google Scholar] [CrossRef] [Scilit]
  166. Spinapolice, E.E. Les Néandertaliens Du Talon: Technologie Lithique et Mobilité Au Paléolithique Moyen Dans Le Salento (Pouilles, Italie Méridionale); Archaeopress Publishing: Oxfordshire, UK, 2018. [Google Scholar]
  167. Crezzini, J.; Boscato, P.; Ricci, S.; Ronchitelli, A.; Spagnolo, V.; Boschin, F. A Spotted Hyaena Den in the Middle Palaeolithic of Grotta Paglicci (Gargano Promontory, Apulia, Southern Italy). Archaeol. Anthropol. Sci. 2016, 8, 227–240. [Google Scholar] [CrossRef] [Scilit]
  168. Rolfo, M.F.; Fiore, I.; Gatta, M.; Ceruleo, P.; Di Francesco, M.; Ferracci, A.; Petronio, C.; Salari, L. The Cave Hyena Den of Grotta Guattari (San Felice Circeo, Central Italy): First Faunal and Environmental Data from the MIS 4 Deposit. Comptes. Rendus. Palevol. 2025, 24, 159–189. [Google Scholar] [CrossRef] [Scilit]
  169. Alhaique, F.; Tagliacozzo, A. L’interpretazione Dei Dati Faunistici Nella Ricostruzione Delle Strategie Di Sussistenza Nel Paleolitico Medio. In Atti del 2° Convegno Nazionale di Archeozoologia, Asti 1997; Abaco Edizioni: Forlì, Italy, 2000; pp. 111–124. [Google Scholar]
  170. Gennai, J.; Higham, T.; Romboni, M.; Fiorillo, A.; Giannì, M.; van der Sluis, L.; Marchi, D.; Starnini, E. Buca Della Iena and Grotta Del Capriolo: New Chronological, Lithic, and Faunal Analyses of Two Late Mousterian Sites in Central Italy. PLoS ONE 2025, 20, e0315876. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  171. Spagnolo, V.; Crezzini, J.; Marciani, G.; Capecchi, G.; Arrighi, S.; Aureli, D.; Ekberg, I.; Scaramucci, S.; Tassoni, L.; Boschin, F. Neandertal Camps and Hyena Dens. Living Floor 150A at Grotta Dei Santi (Monte Argentario, Tuscany, Italy). J. Archaeol. Sci. Rep. 2020, 30, 102249. [Google Scholar] [CrossRef] [Scilit]
  172. Fabbri, P.F.; Panetta, D.; Sarti, L.; Martini, F.; Salvadori, P.A.; Caramella, D.; Fedi, M.; Benazzi, S. Middle Paleolithic Human Deciduous Incisor from Grotta Del Cavallo, Italy. Am. J. Phys. Anthropol. 2016, 161, 506–512. [Google Scholar] [CrossRef] [Scilit]
  173. Arrighi, S.; Freguglia, M.; Ranaldo, F.; Ronchitelli, A. Production and Use in the Lithic Industry of the Mousterian in Santa Croce (Bisceglie, Italy). Hum. Evol. 2009, 24, 91–106. [Google Scholar]
  174. Boscato, P.; Crezzini, J. Modalità Di Sfruttamento Delle Parti Scheletriche Di Bos primigenius Nel Paleolitico Medio e Superiore Della Puglia: Grotta Di Santa Croce (Bisceglie, Bari) e Grotta Delle Mura (Monopoli, Bari). In Atti 5° Convegno Nazionale di Archeozoologia; Edizioni Osiride: Rovereto, Italy, 2010; pp. 39–46. [Google Scholar]
  175. Boscato, P.; Crezzini, J. Il Cavallo e l’Uro: Le Prede Dei Cacciatori Neandertaliani Nella Grotta Di Santa Croce Di Bisceglie (BT). Studi Preist. E Protostoria 2017, 4, 641–646. [Google Scholar]
  176. Marean, C.W. Hunter–Gatherer Foraging Strategies in Tropical Grasslands: Model Building and Testing in the East African Middle and Later Stone Age. J. Anthropol. Archaeol. 1997, 16, 189–225. [Google Scholar] [CrossRef] [Scilit]
  177. Schoville, B.J.; Otárola-Castillo, E. A Model of Hunter-Gatherer Skeletal Element Transport: The Effect of Prey Body Size, Carriers, and Distance. J. Hum. Evol. 2014, 73, 1–14. [Google Scholar] [CrossRef] [Scilit]
  178. O’Connell, J.F.; Hawkes, K.; Jones, N.B. Hadza Hunting, Butchering, and Bone Transport and Their Archaeological Implications. J. Anthropol. Res. 1988, 44, 113–161. [Google Scholar] [CrossRef] [Scilit]
  179. Marin, J.; Saladié, P.; Rodríguez-Hidalgo, A.; Carbonell, E. Neanderthal Hunting Strategies Inferred from Mortality Profiles within the Abric Romaní Sequence. PLoS ONE 2017, 12, e0186970. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  180. Spinapolice, E.E. Neanderthal Mobility Pattern and Technological Organization in the Salento (Apulia, Italy). In Palaeolithic Italy. Advanced Studies on Early Human Adaptations in the Apennine Peninsula; Sidestone: Leiden, The Netherlands, 2018; pp. 95–124. [Google Scholar]
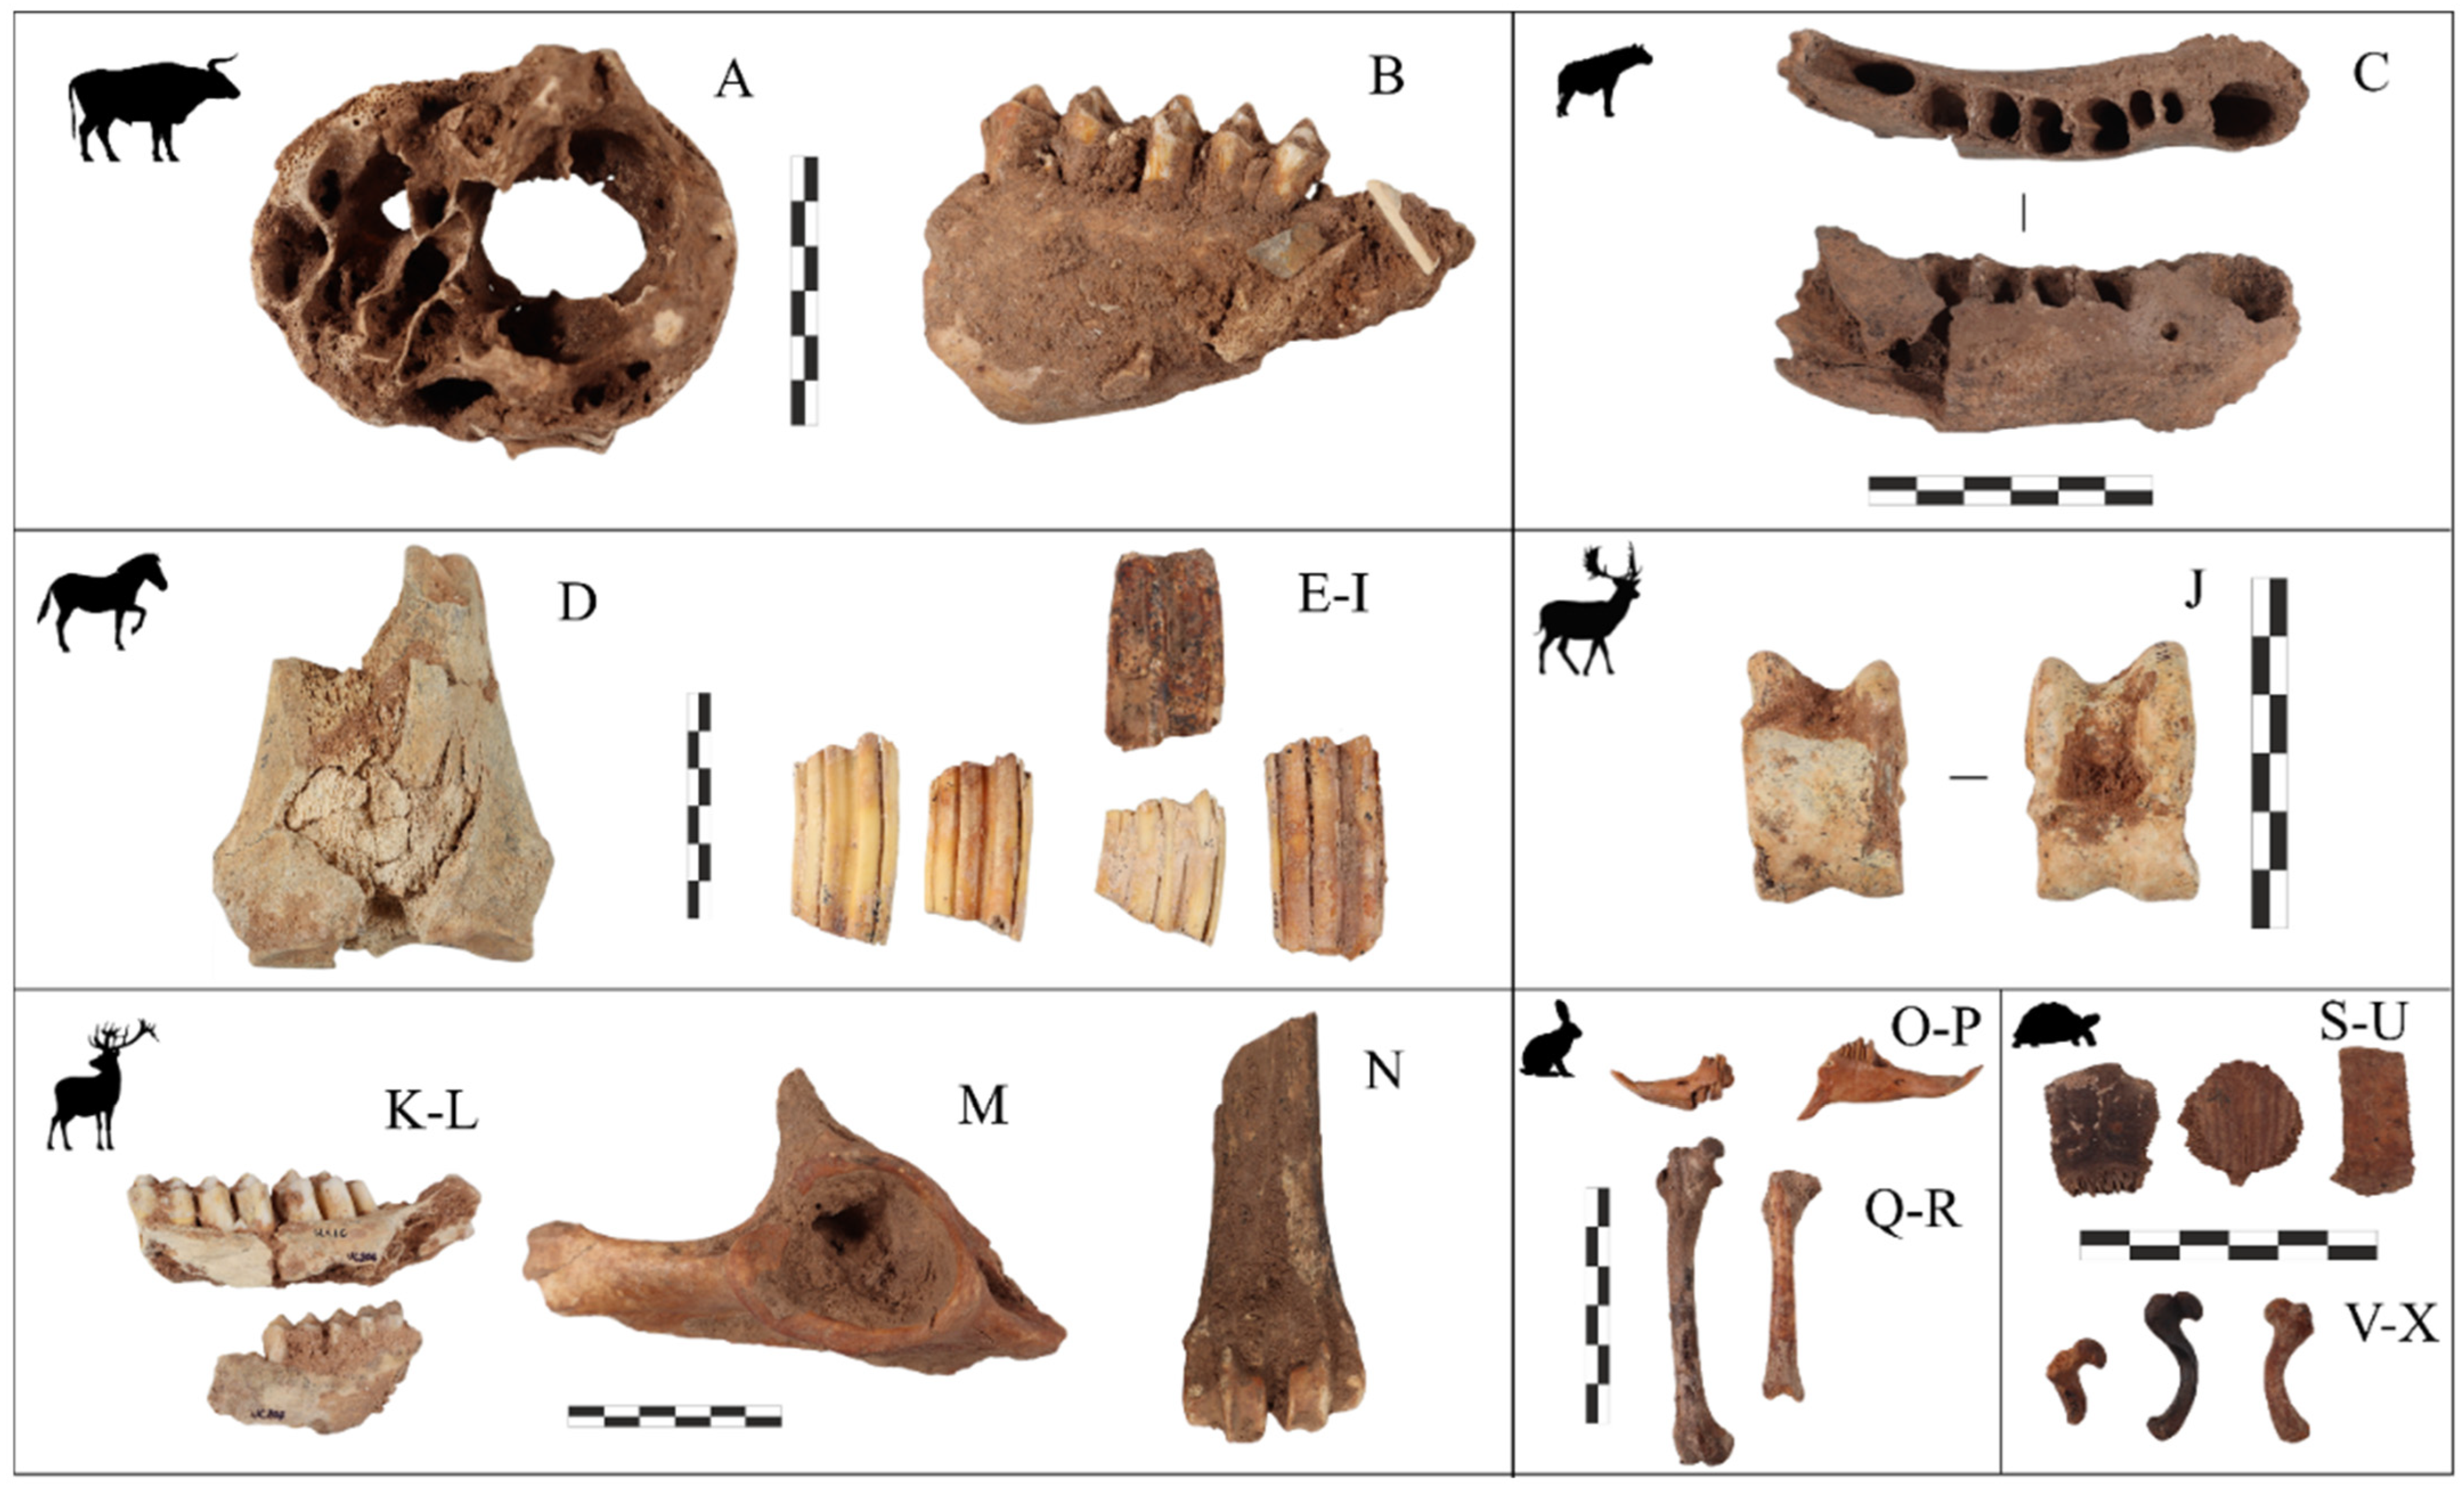
Figure 3. Bone remains from Mousterian layers of Uluzzo C: (A) horn core of Bos/Bison; (B) right hemimandible of juvenile Bos/Bison; (C) right hemimandible of juvenile C. crocuta; (D) right radius of Equus sp.; (E) upper P3 of Equus sp.; (F) lower M2 of Equus sp.; (G) lower M2 of Equus sp.; (H) lower P3 of Equus sp.; (I) lower M3 of Equus sp.; (J) left astragalus of D. dama; (K) left hemimandible of C. elaphus; (L) right hemimandible of juvenile C. elaphus; (M) left pelvis of C. elaphus; (N) left metatarsal of C. elaphus; (O) left hemimandible of Lepus sp.; (P) right hemimandible of Lepus sp.; (Q,R) right femurs of Lepus sp.; (SU) fragments of carapace of Testudo hermanni; (V,W) right humeri of Testudo hermanni; (X) left humerus of Testudo hermanni.
Quaternary 09 00037 g003
Figure 4. Ternary plot of age at death of the ungulate taxa for all three Mousterian layers. Taxa were considered only when the minimum number of individuals (MNI) exceeded four per layer.
Quaternary 09 00037 g004
Figure 5. Bone remains of ungulates with butchery marks from layer G of Uluzzo C: (A) incisions on the hemimandible of C. elaphus; (B) deep striae and incisions on the metatarsal of C. elaphus; (C) consecutive and opposite notches on the metatarsal of D. dama; (D) incisions on the hemimandible of Equus sp.; (E) incisions and scrapings on the hemimandible of B. primigenius.
Quaternary 09 00037 g005
Figure 6. Bone remains of small game with butchery marks from layer G of Uluzzo C. (A) Striated incisions on a pelvis of Lepus sp.; (B) striated incisions on a humerus of Testudo hermanni.
Quaternary 09 00037 g006
Figure 7. Analysis of skeletal composition of Bos/Bison and cervids from layer G according to %MAU.
Quaternary 09 00037 g007
Figure 8. Correlation between %MAU and Bone Volume Density (left) and between %MAU and Marrow Index (right) of cervids from layer G.
Quaternary 09 00037 g008
Table 2. Number of identified specimens (NISP), minimum number of elements (MNE) and minimum number of individuals (MNI) from layers E, F and G of Uluzzo C.
Layer E + SUs 23, 24Layer F + SU 30Layer GTotal Mousterian Layers
NISP%NISPMNEMNINISP%NISPMNEMNINISP%NISPMNEMNINISP%NISP
JSAdAdSJSAdAdF/NBJSAdAdS
Bos primigenius 40.34 1 40.2
Bos/Bison42.82 1121.72 117812.443 214 18410.8
Equus sp.32.12 1 2319.8121 2221.510 121482.8
Cervus elaphus1812.7511213328.414113352.42111 2 865.1
Dama dama74.951 2 1512.99111352.42011 1 573.4
Sus scrofa42.831 1 50.35 1 90.5
Capreolus capreolus10.71 1 65.23 130.22 1 100.6
 Cervidae (size 3-4)2316.2 108.6 60.4 392.3
 Caprinae 10.1 10.06
 Ungulata4431 1311.2 151 724.2
Total Ungulata10473.218317310287.94032830421.110524212151030
Crocuta spelaea10.71 1 20.12 1 30.2
Panthera pardus 20.12 1 20.1
Canis lupus32.11 1 10.11 1 40.2
Vulpes vulpes2114.811 12 766 120.12 1 301.8
Lynx lynx 10.11 1 10.06
Meles meles 10.11 1 10.06
Martes sp.10.71 1 10.06
 Carnivora53.5 10.9 30.2 1 90.5
Total Carnivora3121.814 15 86.96 1120.89 6 513
Lepus sp.10.71 1 20013.915113 16 20111.8
Oryctolagus cuniculus 513.548 1 8 513.0
 Lagomorpha 16411.4 3 10 1649.7
Total Lagomorpha10.71 1 41528.819917 34 41624.5
Testudo hermanni 1147.920 1 6 1146.7
Aves64.2 65.2 59641.4 60835.8
Total identified142100333213311610046329144110033331225811699100
Mammal size 2-3131.3 133.4 20.1 281
Mammal size 4-580.8 51.3 100.7 230.8
Indeterminate80583.2 24664.7 90.6 106037.7
Gran Total968100 380100 1462100 2810100
Table 3. Number of remains showing anthropogenic modifications: cut marks (CM) and percussion marks (PM) with their percentage as butchery marks (%BM) relative to NISP, and thermal alteration (TA).
Anthropogenic Modifications
Layer E+ SUs 23, 24Layer G
NRCMPM%BMTANRCMPM%BMTA
Bos primigenius 4 1
Bos/Bison4 1782 1.149
Equus sp.3 221 4.53
Cervus elaphus181 5.6 352 5.75
Dama dama7 35 12.95.0
Sus scrofa4 5 1
Capreolus capreolus1 3 1
Cervidae (size 3-4)23 6 1
Caprinae 1
Ungulata44 15 2
Crocuta spelaea1 2
Panthera pardus 2
Canis lupus3 1
Vulpes vulpes21 2
Lynx lynx 1 1
Meles meles 1
Martes sp.1
Carnivora5 3
Lepus sp.1 2007 3.536
Oryctolagus cuniculus 51 5
Lagomorpha 1642 1.211
Testudo hermanni 1148 729
Aves6 596
Mammal size 2-313 2
Mammal size 4-58 10 3
Indeterminate805130.5459 1
Total968230.54514622211.6154
Table 4. Number of remains and percentage for the biostratinomic and diagenetic alterations recorded in the Mousterian layers.
Layer E + SUs 23, 24Layer F + SU 30Layer G
NISP%NISPNISP%NISPNISP%NISP
Biostratinomic alterationsRodent marks10.1 211.4
Carnivore marks10.1 171.2
Digestion marks20.251.330.2
Weathering30.3 10.1
Dermestid pupal chambers30.3 70.5
Trampling marks50.5 110.8
Diagenetic alterationsConcretions29530.532585.548933.4
Manganese staining27728.614538.262442.7
Root marks272.8123.218112.4
Corrosion10.130.880.5
Exfoliation 10.360.4
Water dissolution30.3
Total NISP9681003801001462100
Table 5. Taxonomic results obtained from ZooMS analysis for Uluzzo C’s samples by layers.
SpeciesSUsGrand
EF + 30GTotal
Bos/Bison 112
Ungulate 1 1
Total Ungulate 213
Human?1 1
Total determined 213
Indeterminate171221
Grand Total291324
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.