Article

Optimal Dietary Glycerol Monolaurate Supplementation Enhances Growth Performance and Intestinal Health in Hybrid Grouper (♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus)

1
Hainan Provincial Key Laboratory of Tropical Maricultural Technologies, Hainan Academy of Ocean and Fisheries Sciences, Haikou 571126, China
2
The Key Laboratory of Mariculture, Ministry of Education, Ocean University of China, Qingdao 266003, China
3
School of Marine Biology and Aquaculture, Hainan University, Haikou 570228, China
*
Author to whom correspondence should be addressed.
Fishes 2026, 11(9), 519; https://doi.org/10.3390/fishes11090519
Submission received: 21 July 2026 / Revised: 26 August 2026 / Accepted: 27 August 2026 / Published: 2 September 2026

Abstract

This study investigated the effects of glycerol monolaurate (GML) on the growth performance, physiological efficacy, intestinal structure, and microbiota of hybrid juvenile ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. A total of 594 groupers were administered diets supplemented with 0, 2, 4, 6, 8, or 10 g/kg of GML over an 80-day period. The findings indicated that the group receiving 4 g/kg GML supplementation demonstrated significantly enhanced growth performance, as evidenced by increased weight gain, specific growth rate, and a reduced feed conversion ratio compared with the control and other experimental groups. This growth enhancement was associated with elevated catalase and glutathione levels, suggesting improved antioxidant capacity that may contribute to enhanced immune function. Furthermore, fish in the 4 g/kg group exhibited increased digestive enzyme activity and significantly improved intestinal morphology, characterized by thicker muscular layers and a greater fold width and height. Furthermore, compared with the control group, GML supplementation elevated the relative abundance of Proteobacteria while reducing that of Firmicutes at the phylum level. At the genus level, GML markedly suppressed the relative abundance of Mycoplasma and Vibrio. These compositional alterations are potentially linked to improved energy acquisition and a decreased risk of pathogenic infections. Collectively, these results reveal that GML acts as a promising functional feed additive to boost growth performance, optimize digestive capacity, and sustain intestinal structural integrity in hybrid grouper. Based on these results, the optimal GML supplementation dose was determined to be 4 g/kg, providing valuable insights into the role of GML in aquaculture practices for hybrid grouper.
Key Contribution: This study systematically determined that dietary glycerol monolaurate (GML) at an optimal dose of 4 g/kg significantly enhances growth performance, intestinal health, and antioxidant capacity in hybrid grouper, while modulating gut microbiota by reducing potentially pathogenic Vibrio abundance and promoting beneficial bacteria. These findings provide a scientific basis for GML as a sustainable antibiotic alternative in grouper aquaculture, addressing the urgent need for environmentally friendly feed additives to support cleaner production practices.

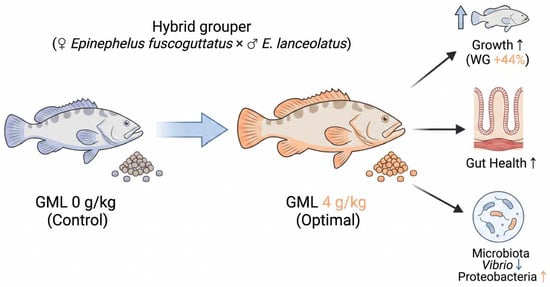
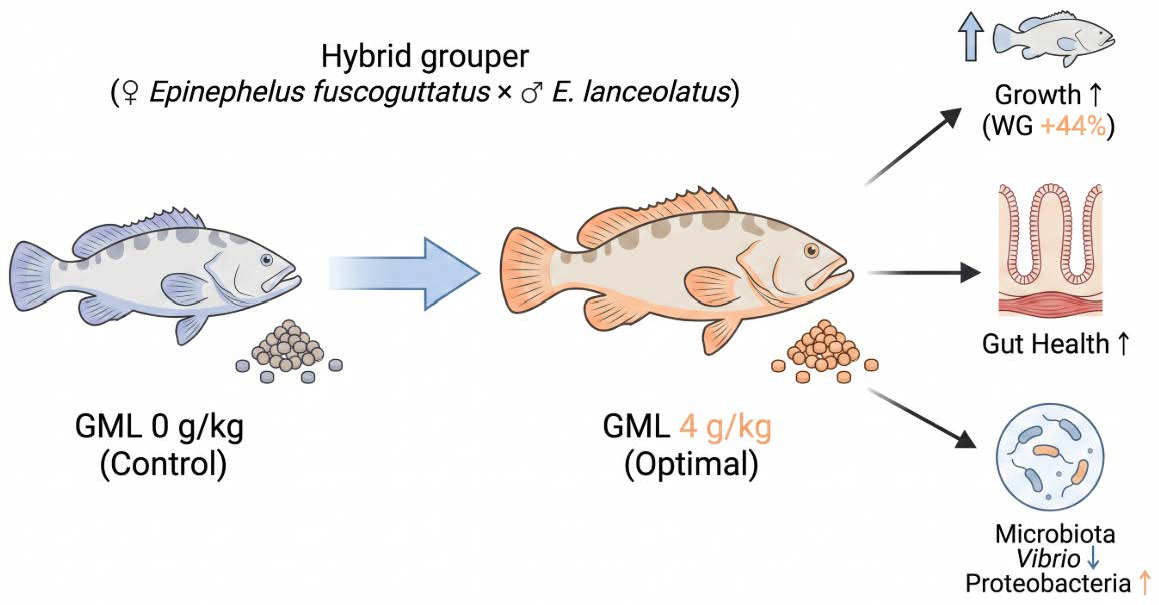
Graphical Abstract

1. Introduction

The hybrid grouper, ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus, commonly called the “pearl gentian grouper”, is known for its high value on the market due to its delicious meat and nutritional richness. Its fast-growing trait also makes it a sought-after choice for aquaculture. Nevertheless, the expansion of farming operations and the intensification of farming practices have led to environmental degradation, resulting in increased disease outbreaks and posing significant challenges to the sustainable development of the grouper farming industry [1]. One promising approach to improving fish’s immune function and disease resistance in aquaculture is the use of natural immunostimulants. These substances can enhance fish and shrimp’s immune response, improving resistance against pathogens and diseases [2]. Natural immunostimulants are generally safe and have no adverse effects on the environment, making them a promising alternative to chemical drugs. Some natural immunostimulants that have been studied in the context of aquaculture include various plant extracts, probiotics, and betaglucans. Plant extracts, such as those from garlic, ginger, and turmeric, have been shown to enhance the immune response of fish and other aquatic species and improve their disease resistance. Probiotics, which are beneficial bacteria that can colonize the fish’s gut, can also enhance immune function and protect against pathogens [3]. Betaglucans, polysaccharides in microorganisms’ cell walls, can stimulate the immune system and enhance disease resistance [4]. As the demand for high-quality and safe seafood continues to increase, developing sustainable and responsible methods for producing fish in aquaculture is essential. Utilizing natural immunostimulants and other strategies to improve fish’s health and disease resistance can play an important role in achieving this goal.
Glycerol monolaurate (GML) is a naturally occurring monoglyceride derived from lauric acid. It is naturally associated with lauric acid-rich sources, including coconut oil and palm-derived plant oils, and it can also be found in human breast milk. GML can be obtained from natural sources or produced through the esterification of glycerol with lauric acid [5,6]. Its natural origin and wide availability make it a promising “green” additive for aquaculture. GML is a promising natural substitute for antibiotics due to its multitude of benefits for animal health. Its non-toxic, harmless, and residual free properties, coupled with its efficient and broad-spectrum antibacterial, antiviral, anti-inflammatory, and other biological activities [7], make GML an appealing option. Additionally, GML has nutritional effects such as energy supply [8].
Recent studies have increasingly investigated GML as a functional feed additive in aquatic animals. Dietary GML supplementation has been reported to improve growth performance, digestive enzyme activities, antioxidant capacity, and nonspecific immune responses in aquatic species. For example, dietary GML supplementation improved growth performance and digestive enzyme activities and enhanced nonspecific immune responses in white shrimp (Litopenaeus vannamei) [8]. In hybrid grouper (Epinephelus fuscoguttatus♀ × E. lanceolatus♂), plant-derived GML supplementation has been reported to improve antioxidant capacity, anti-inflammatory responses, muscle nutritional value, and intestinal microbial composition [9]. These findings suggest that GML may exert beneficial effects on growth, physiological status, and intestinal health in aquaculture species. However, the responses to GML supplementation may vary among species and dietary inclusion levels, and the dose-dependent effects of GML on growth performance and intestinal health in hybrid grouper remain insufficiently characterized.
The metabolic pathway of GML, similar to other medium-chain fatty acids, involves hydrolysis into free lauric acid without emulsification by bile. Lauric acid is rapidly absorbed by small intestinal epithelial cells. It can enter the liver directly via the portal vein through passive diffusion [10], or via transportation by chylomicrons. Once in the liver, it undergoes mitochondrial oxidation, quickly producing energy [11]. Importantly, unlike most antibiotics that target a single bacterial mechanism, GML affects multiple cellular pathways, making it difficult for resistance to develop. The array of benefits GML offers makes it a compelling alternative to antibiotics in animal production, especially in light of increasing concerns about antibiotic resistance.

2. Materials and Methods

2.1. Experiment Diets and Feeding Trial

The basal diet used in the study was provided by Santong Bio-engineering Co., Ltd. in Weifang, China, and its proximate compositions are presented in Table 1. Glycerol monolaurate (GML), supplied by Bio-Form Biotechnology Co., Ltd. in Guangzhou, China, was used as the additive. Six different levels of GML, including 0 (control group), 2, 4, 6, 8, and 10 g/kg, were incorporated into the basal diet. The method of feed pellet production that we utilized was the same as that used in Ding et al.’s study [12]. The feed pellets were placed in plastic bags and stored at −20 °C until usage.
Hybrid groupers averaging 10.15 ± 0.46 g were obtained from the Qionghai Base of the Hainan Academy of Marine and Fishery Sciences in Qionghai, China. A total of 594 fish were randomly allocated to 18,800 L fiberglass tanks (standard aquaculture tanks at the Qionghai Base of the Hainan Academy of Marine and Fishery Sciences, Qionghai, China) and acclimated over 14 days. The experiment, which lasted for 80 days, took place in an outdoor system supplied with filtered seawater, with each tank housing 33 fish. The experimental diets were randomly assigned to triplicate tanks of fish, which were fed twice daily at 08:00 and 17:00 until visual satiation. The amount of feed consumed per tank was recorded. One hour after the feeding, uneaten feeds and feces were removed from the tanks. Daily water quality parameters were closely monitored throughout the experiment to ensure optimal conditions: water temperature was maintained between 25 and 29 °C, pH levels ranged from 7.4 to 8.0, salinity was kept between 28.0 and 31.0 g/kg, dissolved oxygen levels were controlled at 7–8 mg/L, and the ammonia nitrogen concentration was held steady at 0.03 ± 0.01 mg/L. Additionally, 50% of the water was replaced daily. The fish were maintained and fed under natural daylight cycles (14:10, light: dark).

2.2. Proximate Composition and Biochemical Analysis

The proximal compositions of the diet (Table 1), fish body (Table 2), and muscle samples were analyzed using established methods described in previous studies [13]. The nutrient composition of the feed was determined using standard methods. The samples were placed in a ventilated drying oven at 105 °C until a constant weight was reached to determine the moisture content. Moisture content was determined by oven-drying the samples at a constant temperature of 103 °C using an air-blower-driven drying closet (Nocchi Instrument Co., Ltd., Shanghai, China).
Table 2. Compositions of the muscle of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus fed different GML levels.
ParameterFatty Acid Levels (g/kg)
0246810
Moisture75.67 ± 0.176.10 ± 0.176.30 ± 0.176.33 ± 0.176.47 ± 0.177.41 ± 0.1
Crude protein18.48 ± 0.07 d21.70 ± 0.3 a19.73 ± 0.3 b19.63 ± 0.15 bc19.8 ± 0.11 b19.3 ± 0.12 c
Crude lipid1.75 ± 0.05 e2.23 ± 0.02 a2.05 ± 0.05 c2.01 ± 0.02 c1.82 ± 0.02 d2.14 ± 0.02 b
Ash1.41 ± 0.03 c1.53 ± 0.04 b1.71 ± 0.03 a1.11 ± 0.02 d0.91 ± 0.01 e0.88 ± 0.02 e
Data are presented as mean ± SD. Data marked with different letters differed significantly (p < 0.05) among treatments. The same as below.
The crude protein content, expressed as nitrogen multiplied by 6.25, was determined using a rapid N exceed instrument (Elementar Co., Ltd., Langensebold, Germany). Ash content, representing the inorganic mineral content, was quantified by combusting the samples at 550 °C in a muffle furnace (Laboratory Instrument Co., Ltd., Shanghai, China). Crude lipid content, expressed as a percentage of the dry weight, was determined using ether extraction with a Soxtec System (Zhejiang Tuopu Instrument Co., Ltd., Zhejiang, China). By employing these standardized methods, the nutrient compositions of the diet and muscle samples were accurately determined, allowing for further analysis and evaluation of their nutritional profiles.

2.3. Histological Analysis

The proximal (PI), intermediate (MI), and distal intestine (DI) sections samples were collected from three fish per tank for histological analysis. These gut sections were initially immersed in a 4% paraformaldehyde solution and fixed for 24 h to preserve their structural integrity. They were then transferred to 70% ethanol for further preservation. Subsequently, the samples underwent dehydration using graded concentrations of ethanol (70%, 80%, 90%, 95%, and 100%) and were then treated with xylene solution for clarification. Afterward, they were embedded in paraffin wax. Sections of 5–7 μm thickness were cut, stained with hematoxylin and eosin, and then sealed with neutral gum. Observations were made under an inverted microscope at a magnification of 100 times. Image acquisition software was used to measure the fold height (PH), fold width (PW), and muscular thickness (MLT) of the samples.

2.4. Enzymatic Assays

The intestinal samples were rinsed with precooled 0.9% normal saline and dried using filter paper. A weight of 0.4 g of sample was mixed with 0.9% normal saline in a ratio of 1:9 (weight to volume) and subjected to homogenization. The resulting homogenate was then centrifuged at 2500× g for 10 min at 4 °C. The supernatant was collected and stored at −80 °C until further analysis. Biochemical analyses were conducted using commercial test kits from the Nanjing Jiancheng Institute of Biological Engineering (Nanjing, China). The analyses included trypsin activity (TPS, NO. A080-2-2), amylase activity (AMY, NO. C016-1-1), lipase activity (LIP, NO. A054-2-1), superoxide dismutase activity (SOD, NO. A001-3-2), alanine aminotransferase activity (ALT, NO. C009-2-1), catalase activity (CAT, NO. A007-2-1), glutathione peroxidase content (GSH-Px, NO. A006-2-1), and malondialdehyde content (MDA, NO. A003-1-2). All assays were performed in triplicate, following the manufacturer’s instructions.

2.5. Serum Biochemical Parameter Analysis

Blood samples were collected from the caudal vein using a 1 mL sterile syringe and allowed to sit at room temperature for 4 h. The samples were then centrifuged at 3500× g for 10 min at 4 °C. The supernatant was carefully collected and stored at −80 °C for further analysis. To analyze the serum biochemical parameters, a PUZS-300 automatic biochemical analyzer (Perlong New Technology Co., Ltd., Beijing, China) was used following the manufacturer’s instructions. Reagents from Randox Laborato-ries Ltd. (Northern Ireland, UK) were utilized for the detection of albumin (ALB), triglyceride (TG), total cholesterol (CHO), total protein, creatinine (CRE), high-density lipoprotein (HDL-C), low-density lipoprotein (LDL-C), urea, and calcium (Ca).

2.6. Gut Microbiota Structure Analysis

Total DNA was extracted from microbial community samples collected from the guts using the CTAB method and analyzed at Lianchuan Biotechnology Co., Ltd. (Hangzhou, China). PCR amplification was performed using the forward primer 341F (5′-CCTACGGGNGGCWGCA-3′) and the reverse primer 805R (5′-GACTACHVGGGTATCTAATCC-3′). Samples were analyzed using an Agilent 2100 Bioanalyzer (Agilent, Santa Clara, CA, USA) and the Illumina Library Quantification Kit from Kapa Biosciences (Woburn, MA, USA). Sequencing was performed using a NovaSeq 6000 sequencer with a NovaSeq 6000 SP Reagent Kit for 2 × 250 bp paired-end sequencing (500 cycles) (Illumina, Inc., San Diego, CA, USA).

2.7. Calculations

After the feeding trial, growth performance, feed efficiency, and survival were evaluated using the following parameters:
Weight   gain   ( WG ,   % )   =   100 × W f   W i W i
Condition   factor   ( CF ,   g / cm 3 ) = 100 ×   Body   w e i g h t   ( Body   length ) 3
Specific   growth   rate   ( SGR ,   % / d ) = 100 × [ ln   ( W f )     ln   ( W i ) ] Δ T
Feed   conversion   ratio   ( FCR ) = Dry   feed   fed W f W i
Survival   rate   ( SR ,   % ) = 100 × N f   N i
Wf: final body weight; Wi: initial body weight; Nf: final number of fish; and Ni: initial number of fish.

2.8. Statistical Analysis

Data were presented as mean ± standard deviation (SD). Statistical analyses were performed using PASW Statistics (ver. 18). Levene’s test was used to assess the homogeneity of variances. Because dietary GML was supplied at six quantitatively ordered levels (0, 2, 4, 6, 8, and 10 g/kg), linear and quadratic regression analyses and orthogonal polynomial contrasts were performed to evaluate the dose-dependent effects of GML supplementation on growth performance, feed efficiency, and survival. For other measured parameters, one-way analysis of variance (ANOVA) followed by an appropriate multiple-comparison test was used to assess differences among dietary treatments. Percentage data were appropriately transformed when necessary to satisfy the assumptions of the statistical analysis. Statistical significance was accepted at p < 0.05.
Species diversity analysis, classification annotation, and differential analysis were conducted using the sequencing platform. The correlation between microbial abundance and changes in aquaculture water and grouper intestines was calculated. Based on specific screening conditions, Spearman correlation analysis was used to determine the relationship between the top 30 most abundant microbial genera. The significance (p-value) of the correlations was calculated, and a correlation heatmap was generated for further analysis.

3. Results

3.1. Growth Performance, Feed Efficiency, and Survival of Fish

In the present study, the experimental groups demonstrated superior growth performance compared to the control group to a certain extent (Table 3). Although the initial body weight (IBW) across treatments was similar (approximately 10 g), the final body weight (FBW) increased with fatty acid levels, reaching the highest mean (221.35 ± 8.40 g) at 4 g/kg, which was significantly different from other groups (p < 0.05). Weight gain exhibited a nonlinear response to dietary GML supplementation, increasing with GML inclusion up to 4 g/kg and subsequently decreasing at higher inclusion levels. Regression analysis revealed a significant quadratic relationship between dietary GML concentration and weight gain (p < 0.05), indicating an intermediate dose associated with maximal growth performance. The estimated optimum was approximately 4 g/kg GML.
The CF was highest at 0 and 2 g/kg (2.06 ± 0.65 and 2.11 ± 0.35, respectively) but decreased at 10 g/kg (1.58 ± 0.22), suggesting that very high GML levels may reduce body robustness. Specific growth rate showed a significant quadratic response to dietary GML supplementation (p < 0.05), with SGR increasing up to the intermediate GML level and subsequently declining at higher supplementation levels. Feed conversion ratio exhibited a significant dose-dependent response to dietary GML supplementation, with FCR decreasing at intermediate GML levels and increasing thereafter. The significant quadratic response indicated improved feed utilization at an intermediate GML inclusion level (p < 0.05), and the FCR improved (lower values) with increased GML levels, reaching optimal values at 4–6 g/kg, showing efficient feed utilization at these levels. Survival rate showed a nonlinear response to dietary GML supplementation, with the highest observed value at 4 g/kg. Orthogonal polynomial contrast analysis was used to assess the linear and quadratic components of the dose–response relationship. A significant quadratic effect was detected (p < 0.05), indicating that survival was maximized at an intermediate GML supplementation level. Overall, the results suggest that 4 g/kg GML provides the most favorable balance for growth, feed efficiency, and survival.

3.2. Muscle Compositional Parameters of Fish

The analysis of muscle moisture content revealed no significant impact from GML supplementation (p > 0.05, Table 2). However, the muscle crude protein content exhibited a significant association with GML levels (p < 0.05). The highest body crude protein content was observed in the 2 g/kg group. Additionally, different GML levels exerted an important influence on muscle lipid content. Specifically, the 2 g/kg group exhibited the highest muscle lipid content, while the control group showed the lowest. Regarding ash content, the highest value was observed in the 4 g/kg group, with the lowest in the 8 g/kg group and 10 g/kg group.

3.3. Intestinal Morphology of Fish

The examination of the integrity and morphology of the different intestine sections showed that all experimental groups exhibited intact intestines (Figure 1). Consistent muscle thickness, plica height, and plica width without any signs of damage or injury were observed in all treatments (Table 4). Thorough analysis revealed that GML levels had a significant effect on the thickness of the muscular layer (p < 0.05). Particularly, the muscular layer thickness in PI showed a significant increase in the 10 g/kg group, exceeding all other groups (p < 0.05). In contrast, the muscular layer thickness of MI and DI initially increased and then decreased, reaching their peak values in the 4 g/kg and 6 g/kg groups, respectively. Regarding plica height, GML levels also exerted a significant influence on PI and DI (p < 0.05). Notably, the highest plica in the PI was observed in the 10 g/kg group, while the DI exhibited the most significant plica height in the 4 g/kg group. Furthermore, GML significantly affected the plica width (p < 0.05), with the PI 4 g/kg group displaying notably higher values than other groups. Conversely, as the level of GML increased, the fold width of the DI and MI decreased. It is worth mentioning that the control group exhibited the highest plica width among all the experimental groups (p < 0.05).

3.4. Enzymatic and Antioxidant Activity

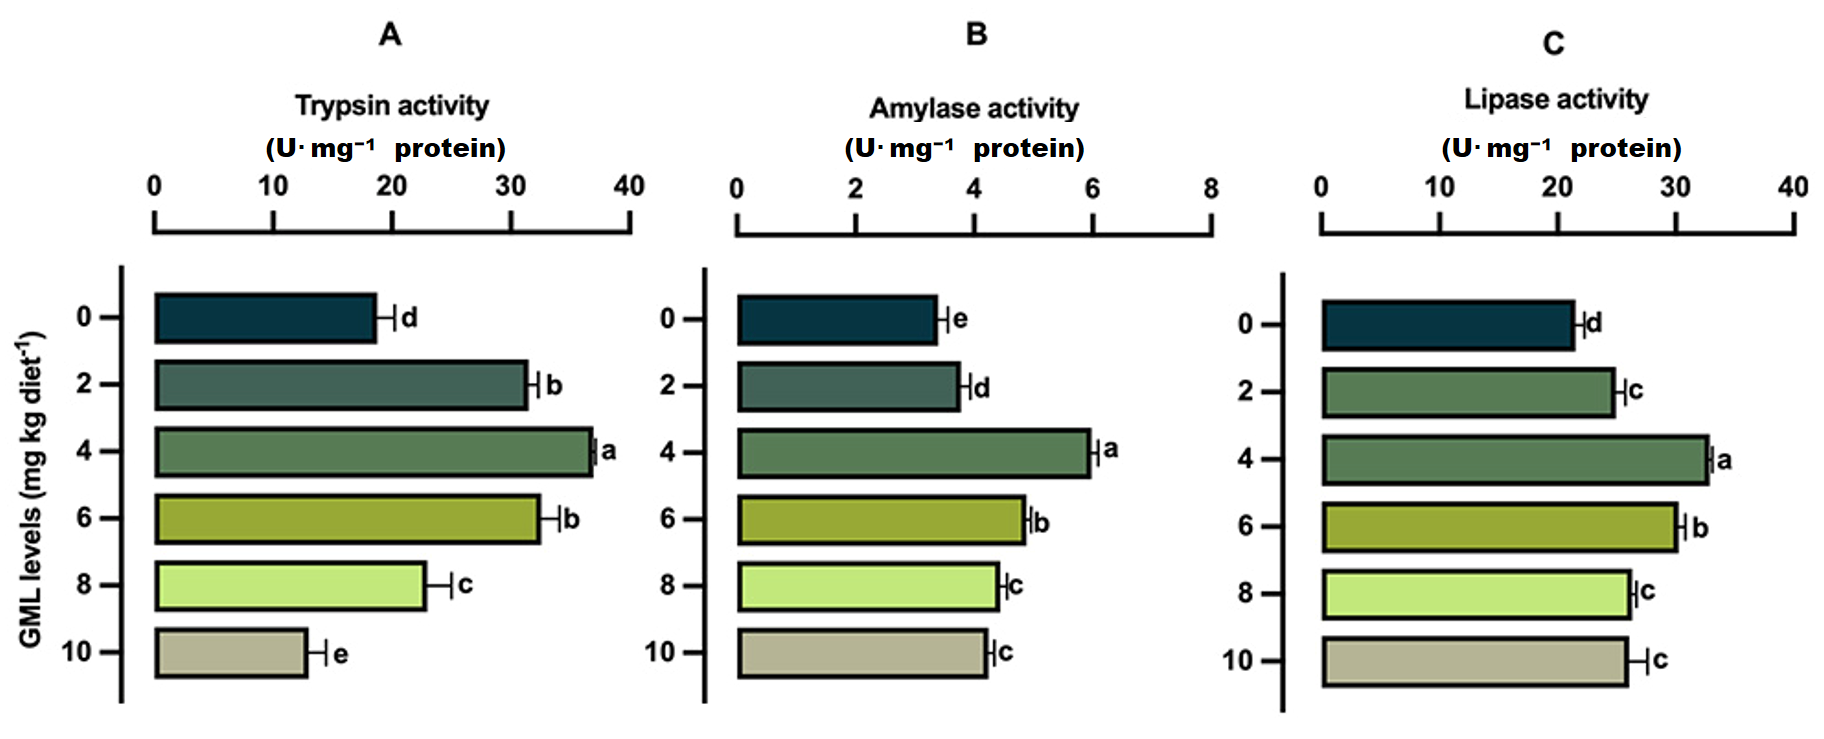
GML supplementation significantly influenced enzymatic activity in the hybrid fish, particularly TPS, AMY, and LIP activities (p < 0.05). TPS activity varied across dosage groups, with the 4 g/kg group exhibiting significantly higher activity than all other groups (p < 0.05, Figure 2A). AMY and LIP activities were also significantly higher in the supplemented groups compared to the control (p < 0.05, Figure 2B,C). AMY and LIP activity peaked in the 4 g/kg group, while the control group exhibited the lowest activity. It is noteworthy that the 10 g/kg group consistently showed lower activity than the highest levels achieved across treatments within all enzymes. Specifically for TPS, activity in the 10 g/kg group was even lower than in the control group.
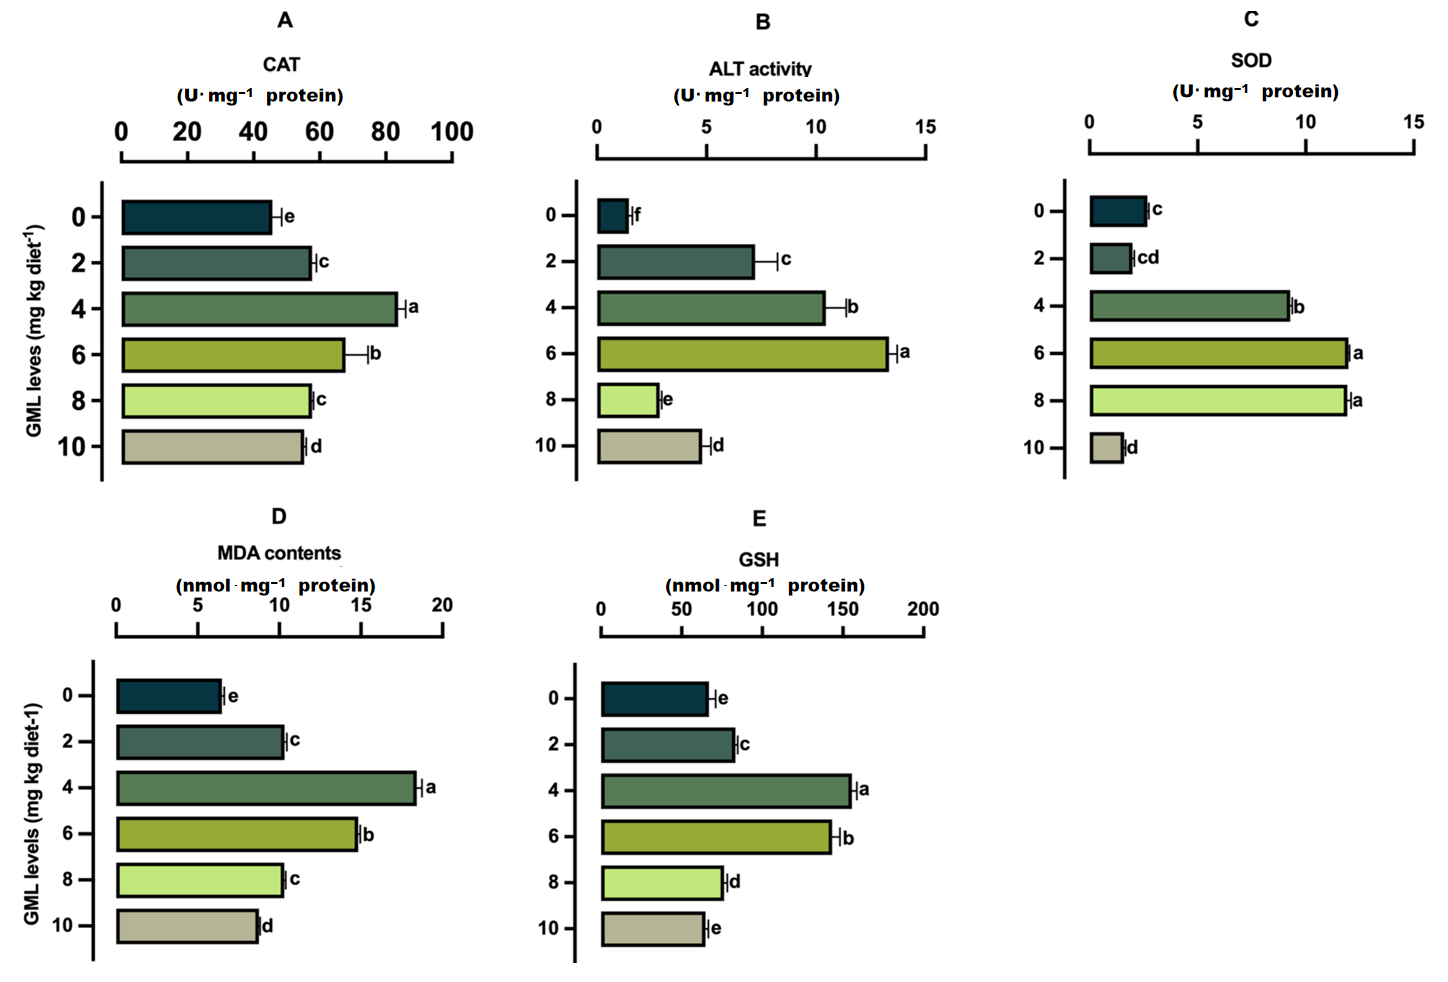
All groups supplemented with GML, except for SOD, displayed an initial rise followed by a decline in antioxidant activity with increasing GML levels (Figure 3). The peak activity of most enzymes was observed in groups receiving 4 g/kg or 6 g/kg of GML. CAT, MDA, and GSH levels followed a clear bell-shaped trend across treatments, with the 4 g/kg group exhibiting significantly higher values than the other supplemented groups (p < 0.05). ALT activity peaked in the 6 g/kg group, followed by a significant drop in the 8 g/kg group (p < 0.05) and a partial rebound at 10 g/kg, which remained higher than the control but did not reach the peak observed at 6 g/kg. For SOD, initial activity at 2 g/kg was not significantly different from the control. At 4 g/kg, SOD activity increased sharply, reaching a plateau in the 6 g/kg and 8 g/kg groups with no significant difference between these two doses (p > 0.05). However, the 10 g/kg group showed a sudden and significant decrease in activity (p < 0.05). MDA levels, indicative of lipid peroxidation, were lowest in the control (0 g/kg) group. The highest levels were recorded in the 4 g/kg group, while the 2 g/kg, 8 g/kg, and 10 g/kg groups showed intermediate levels. Elevated MDA levels were also observed in the 6 g/kg group. GSH levels were significantly higher in the 4 g/kg group, closely followed by the 6 g/kg group. The lowest levels were recorded in the control and 10 g/kg groups, while intermediate levels were observed in the 2 g/kg and 8 g/kg groups. Notably, there was no significant difference in GSH levels between the 10 g/kg group and the control (p > 0.05).

3.5. Serum Biochemical Parameters

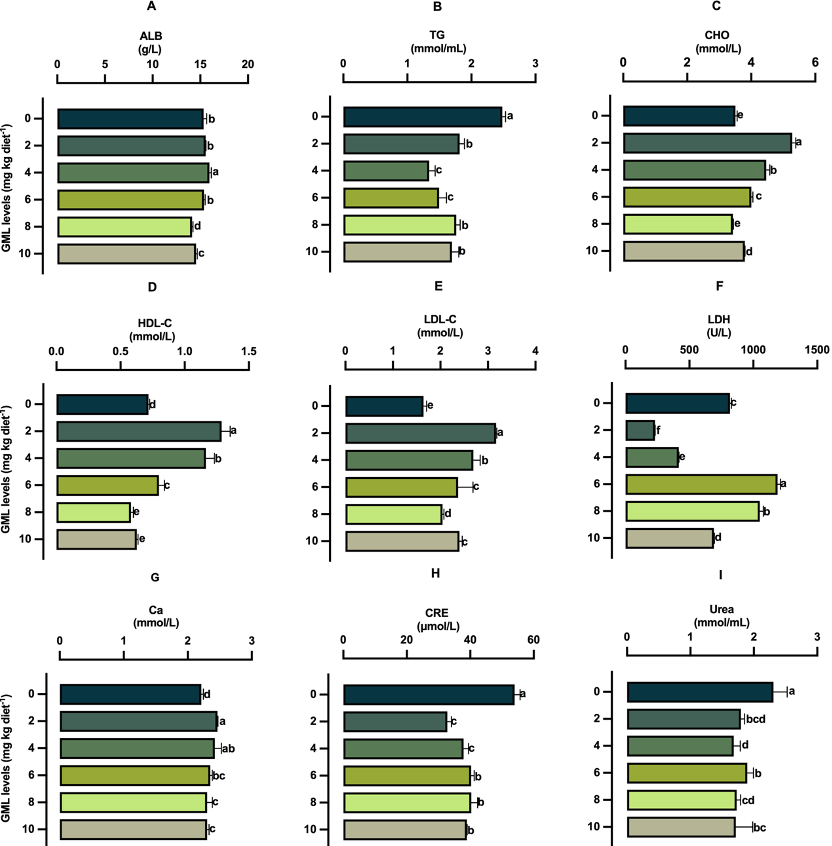
The serum biochemical parameters of hybrid fish were significantly influenced by GML supplementation (Figure 4). ALB levels (Figure 4A) exhibited a significant increase at the 4 g/kg treatment (p < 0.05) but declined thereafter, with the lowest levels observed at 8 and 10 g/kg, falling below those of the control group. In contrast, TG levels (Figure 4B) showed a consistent decline with increasing GML concentrations (p < 0.05). The control group exhibited the highest TG levels, while the lowest levels were observed in the 4 and 6 g/kg groups, followed by a slight increase at 8 and 10 g/kg. CHO, HDL-C, and LDL-C levels (Figure 4C–E) also decreased in a dose-dependent manner. The 2 g/kg group had the highest values for these parameters, but the levels progressively declined with higher GML supplementation, with 8 and 10 g/kg showing the lowest concentrations (p < 0.05). LDH activity (Figure 4F) showed a more variable trend. The lowest activity was observed in the 2 g/kg group, followed by an increase peaking at 6 g/kg. LDH levels then dropped again at 8 and 10 g/kg. For Ca (Figure 4G), there was a general decline with increasing GML levels, though differences among groups were less pronounced compared to other parameters. CRE levels (Figure 4H) decreased significantly in a dose-dependent manner (p < 0.05), with the lowest concentrations observed at 2 and 4 g/kg. These levels appeared to stabilize at higher GML concentrations but remained below those of the control group. Similarly, urea levels (Figure 4I) showed a significant reduction across all GML treatments (p < 0.05), though no clear dose-dependent trend was evident among the treatment groups. Overall, GML supplementation demonstrated distinct effects on serum biochemical parameters, with notable dose-dependent reductions in several key markers and variability in others, emphasizing the nuanced physiological impact of GML on fish metabolism.

3.6. Microbiota of Fish Gut and Aquaculture Water

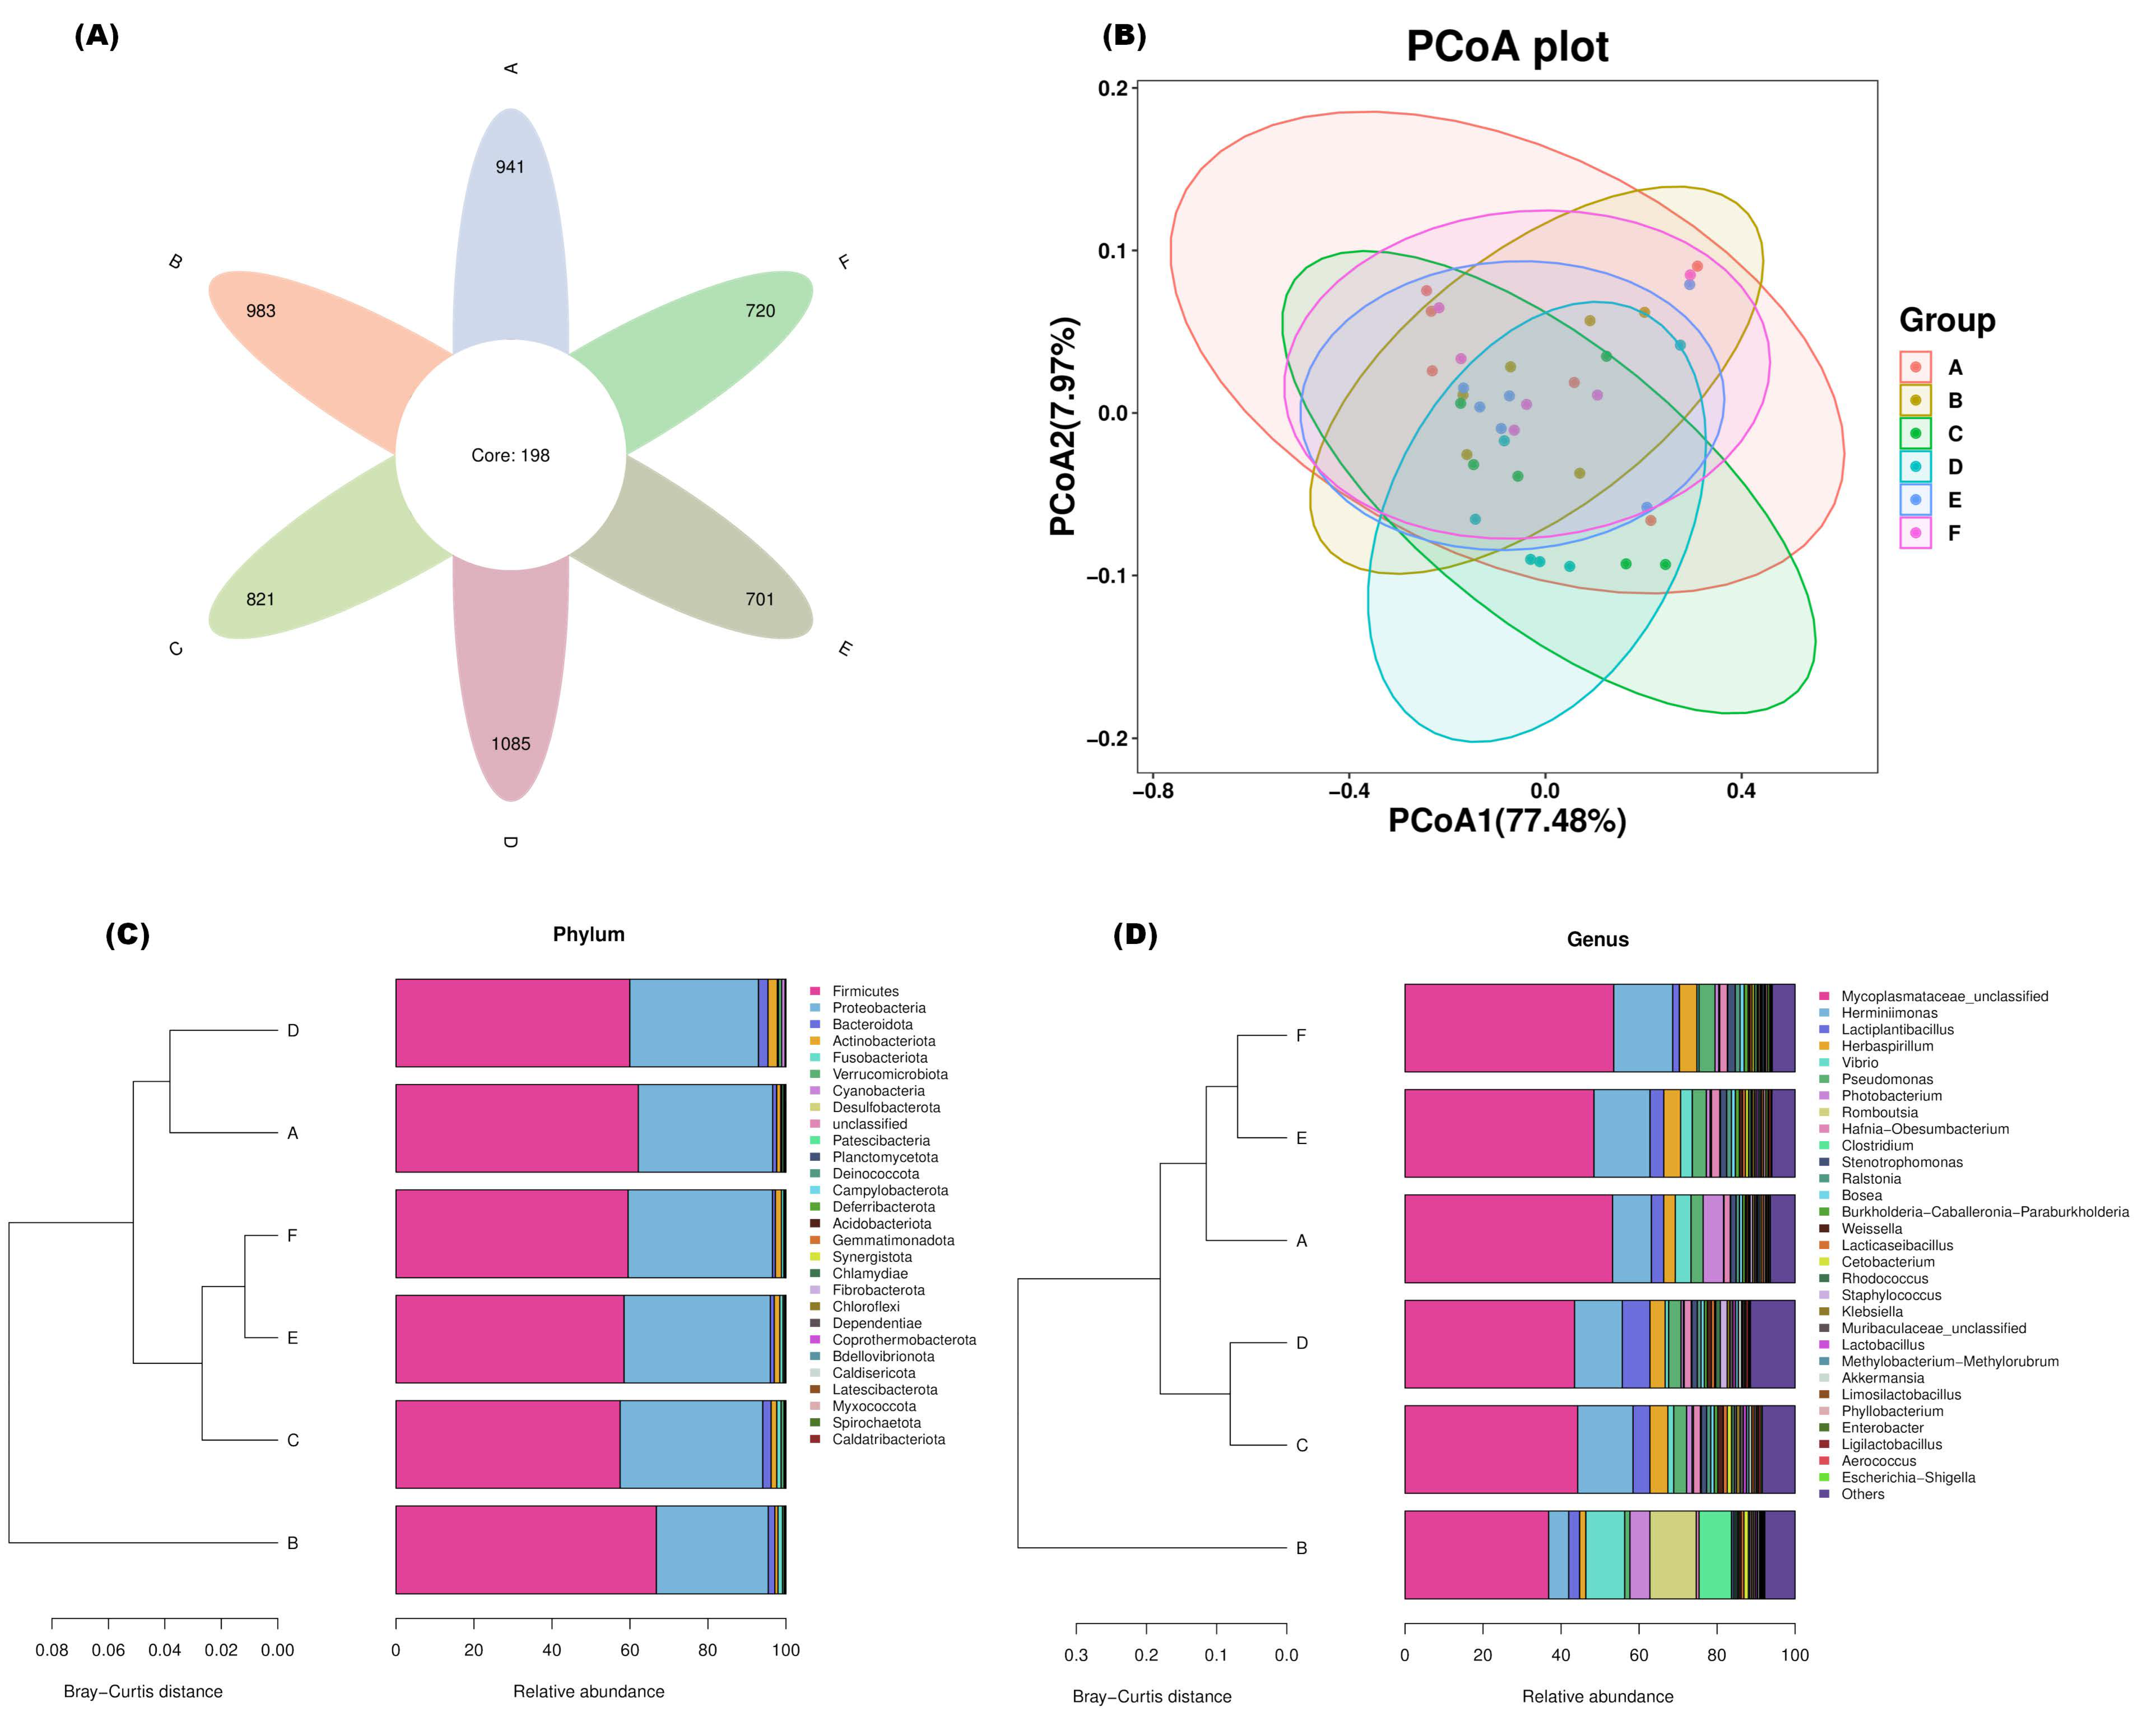
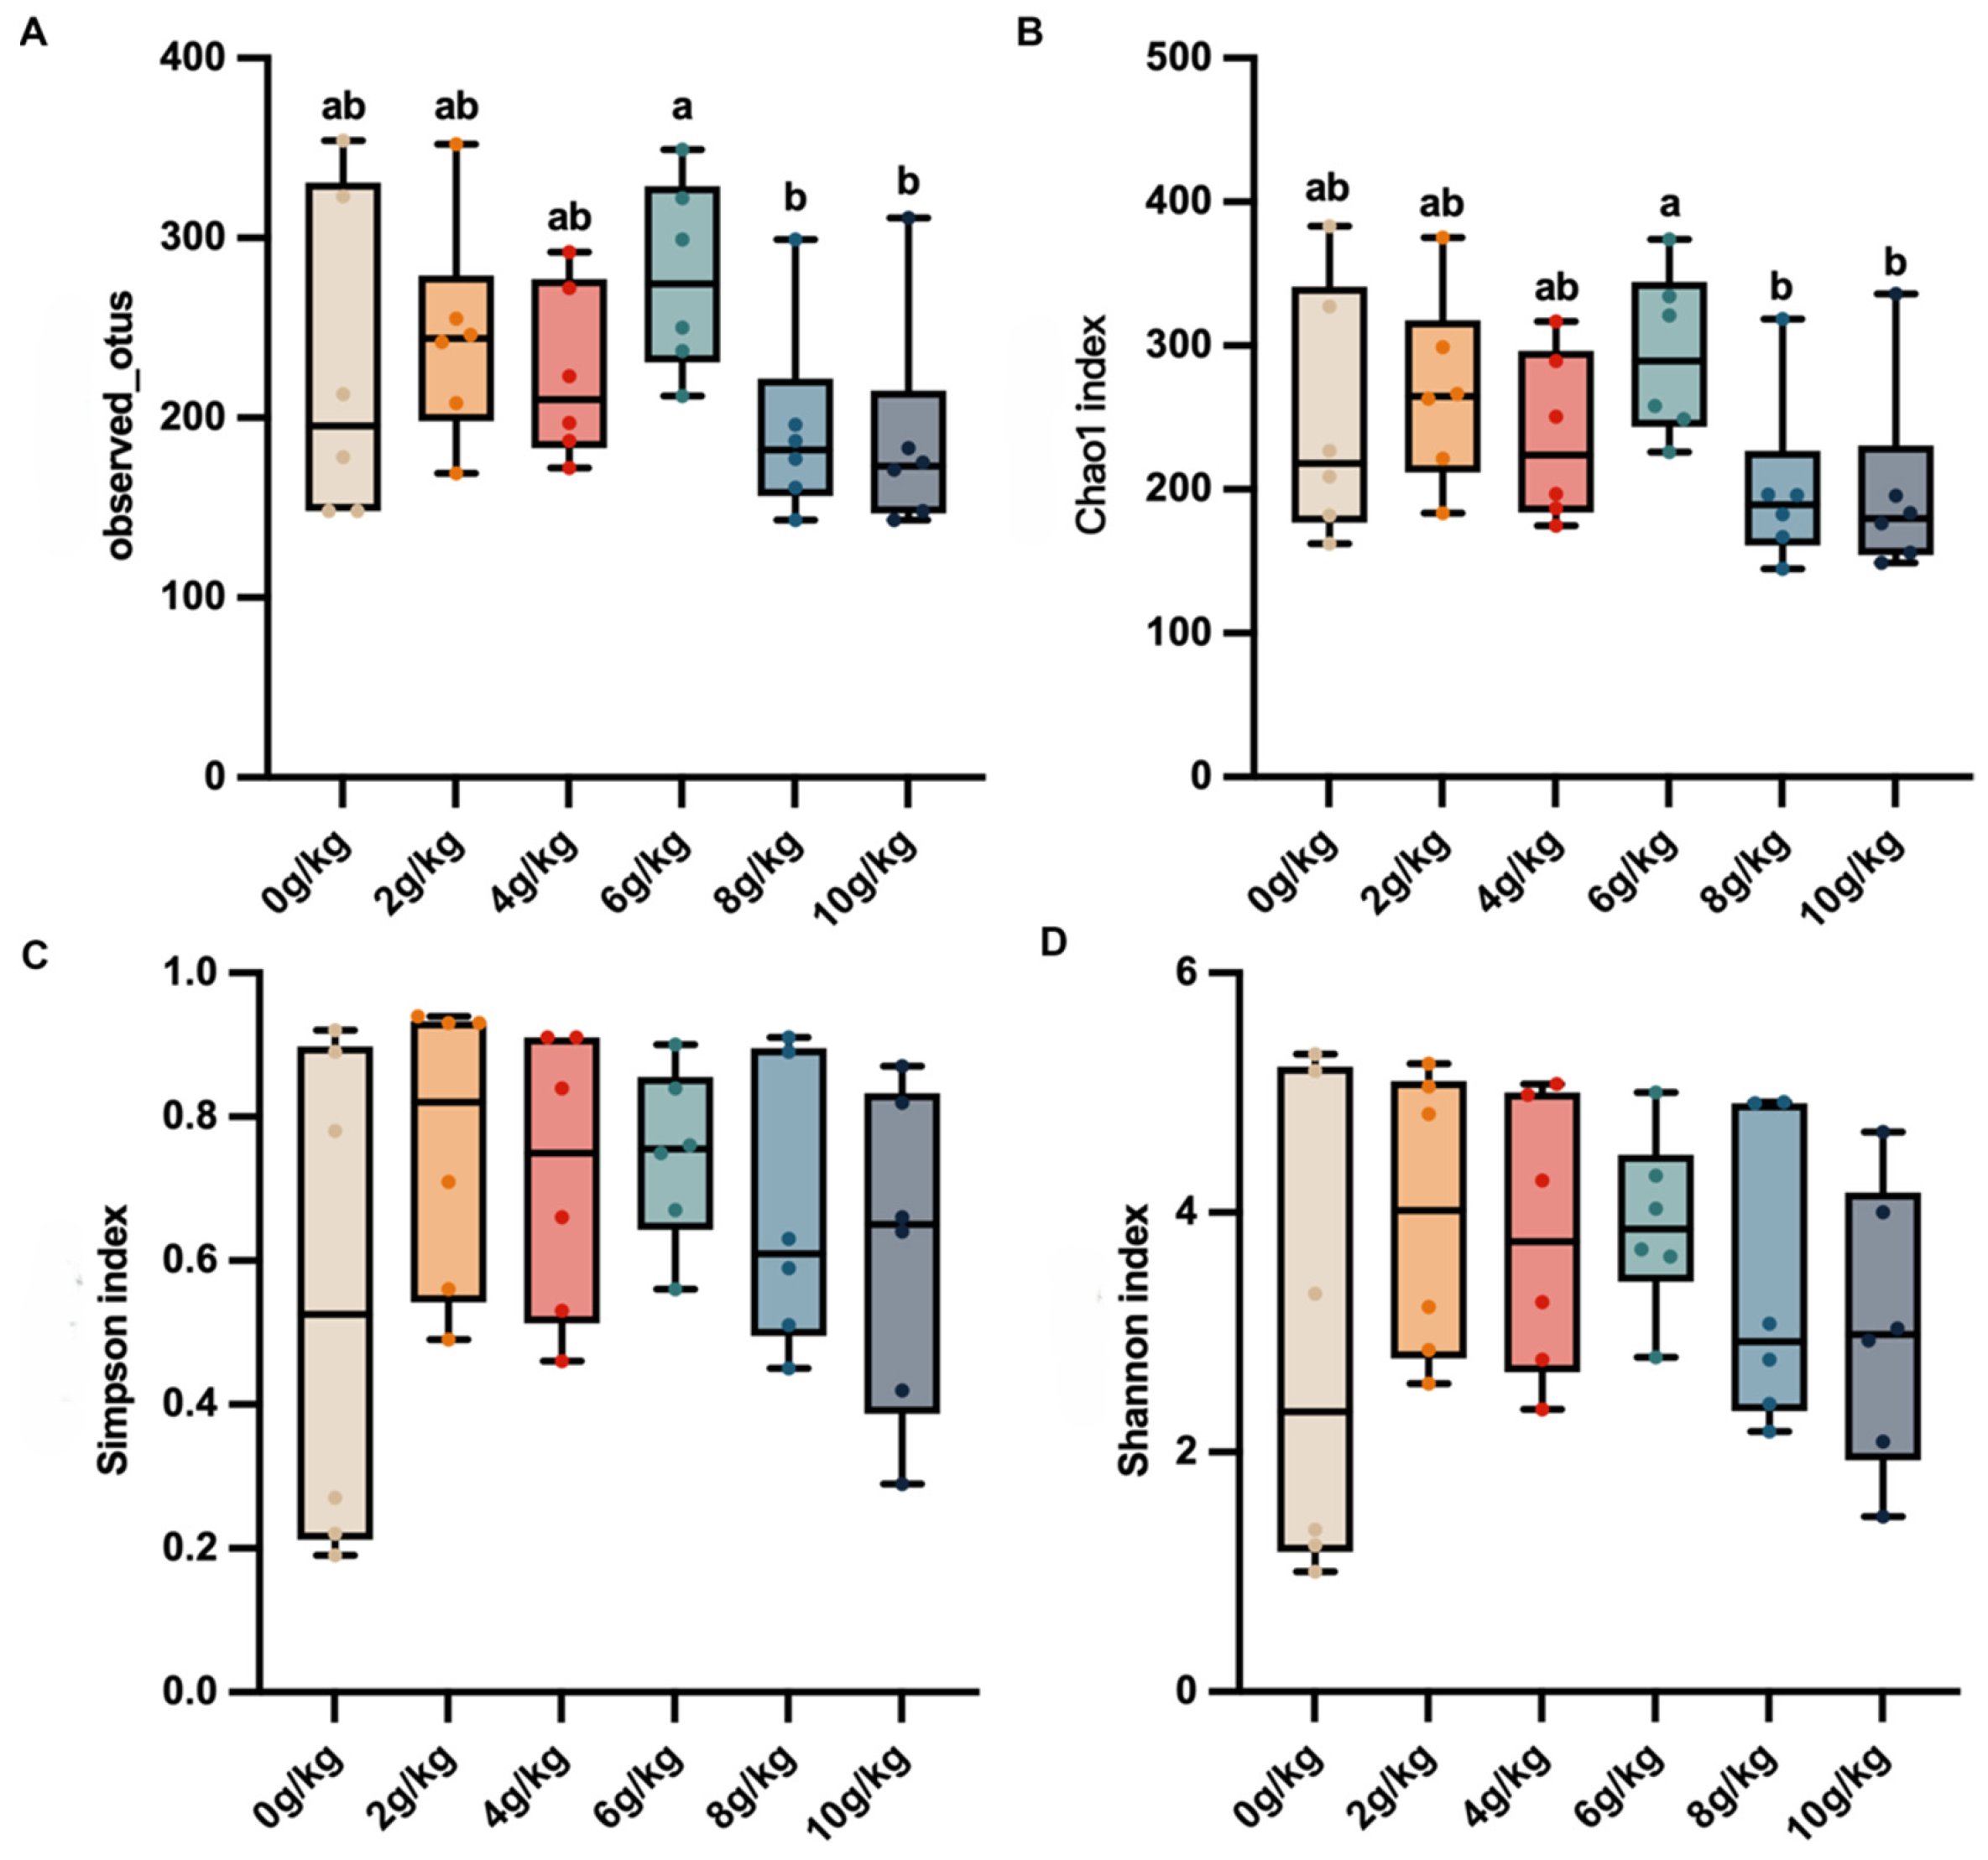
By analyzing microbial sequences of the hybrid fish gut, we classified sequences with 97% similarity into the same category. The Venn diagram indicated that the six groups shared 198 OTUs, while the number of unique OTUs in the 0, 2, 4, 6, 8, and 10 g/kg groups was 941, 983, 821, 1085, 701, and 720, respectively (Figure 5A). Additionally, principal coordinate analysis (PCoA) was used to examine the differences in species composition and structure among the samples. The results showed no clear separation between the control and experimental groups, with the first and second principal coordinates accounting for 77.48% and 7.97% of the total variance, respectively (Figure 5B). In terms of microbial community composition, Firmicutes and Proteobacteria were the most abundant phyla, with Firmicutes accounting for over 57% in each group. The abundance of Proteobacteria increased, while Firmicutes decreased after GML addition (Figure 5C). At the genus level, the five most abundant genera were Mycoplasma, Herminiimonas, Lactiplantibacillus, Herbaspirillum, and Vibrio. Compared to the control group, the relative abundance of dominant genera shifted in the GML-supplemented groups (Figure 5D). In the alpha diversity analysis (Figure 6), we observed that as the level of monolaurin (GML) increased, the number of Operational Taxonomic Units (OTUs) and species richness index peaked in the 6 g/kg group. Although there were no statistically significant differences between the 0, 2, 4, and 6 g/kg groups (p > 0.05), the OTU counts were significantly higher than in the 8 and 10 g/kg groups (Figure 6A, p < 0.05). However, the Shannon and Simpson indices showed no significant differences among the groups (Figure 6C,D; p > 0.05).
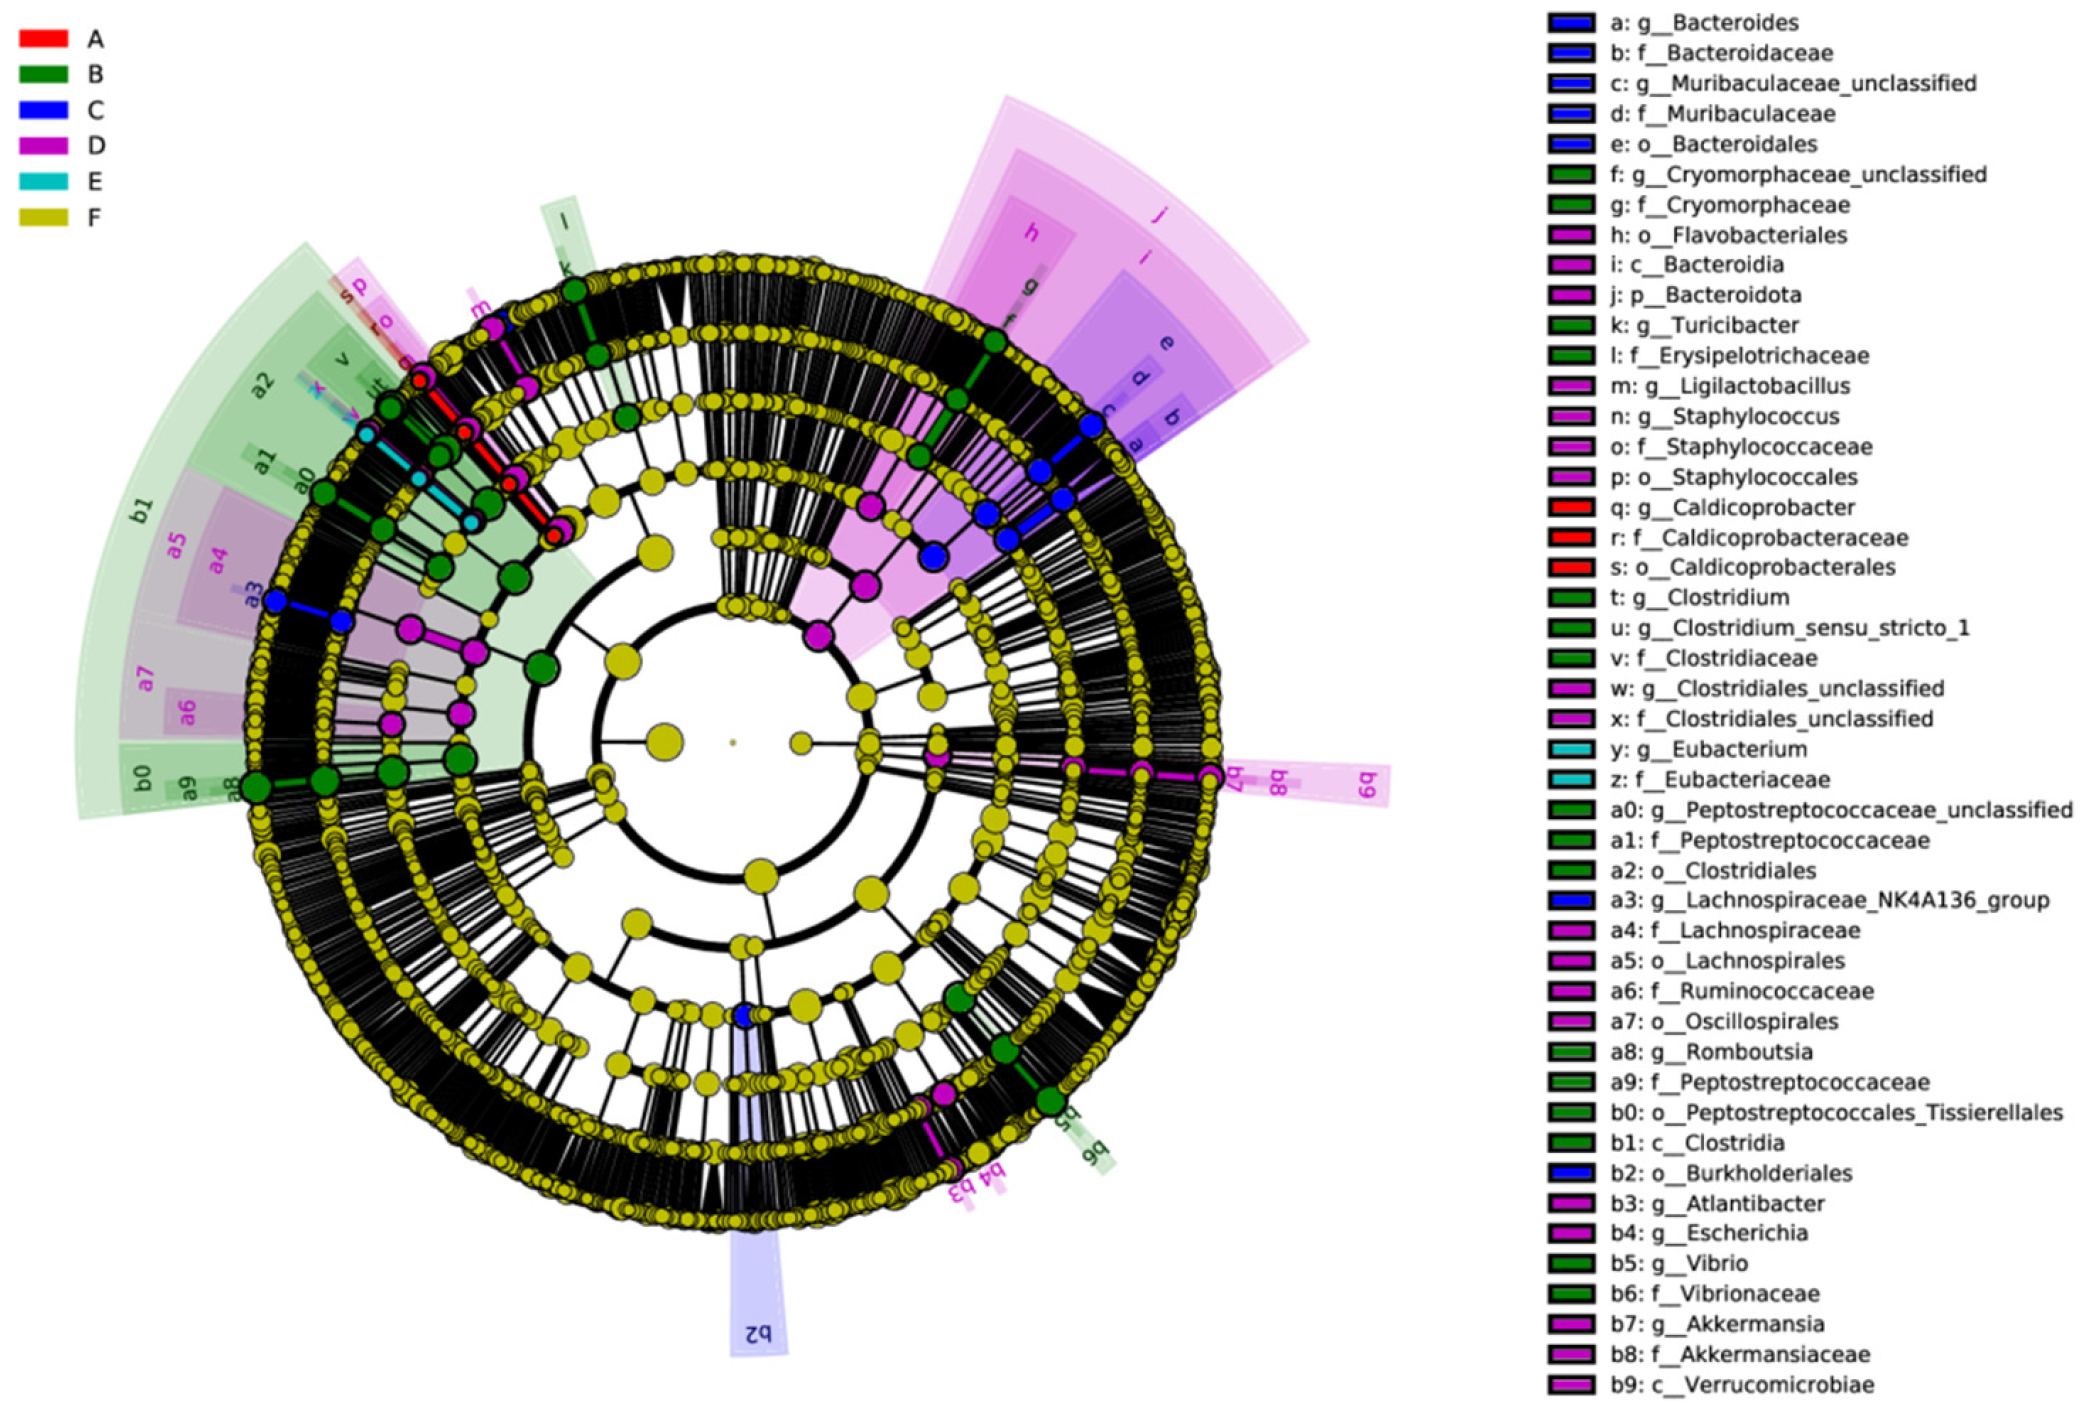
To further explore the microbial composition differences, we conducted a Linear Discriminant Analysis Effect Size (LEfSe) analysis (Figure 7). The results indicated that the control group had three distinct microbial taxa, whereas the 2, 4, 6, and 8 g/kg groups had 16, 7, 18, and 2 distinct microbial taxa, respectively. Notably, the 10 g/kg group did not show any distinct microbial taxa.
Microbial function predictions in the hybrid grouper gut microbiota were made using PICRUSt2. Welch’s t-test was used to analyze differences in gut microbiota KEGG pathway abundance among the groups. At KEGG Level 1, most functional categories were associated with metabolism and genetic information processing. At KEGG Level 2, replication and repair (8.6%) and translation (5.4%) were the two most enriched functions (p < 0.05). However, no significant functional differences were found among the treatment groups (p > 0.05). Further analysis at KEGG Level 3 identified a total of 293 KEGG pathways across all samples. When analyzing the top 50 most abundant pathways, the 8 g/kg group showed a significantly higher enrichment of functional genes related to the Vibrio cholerae pathogenic cycle compared to the other five groups (p < 0.05). Additionally, KEGG Level 3 pathway analysis revealed significant enrichment in vitamin B6 metabolism and Vibrio cholerae pathogenic cycle pathways (p < 0.05).
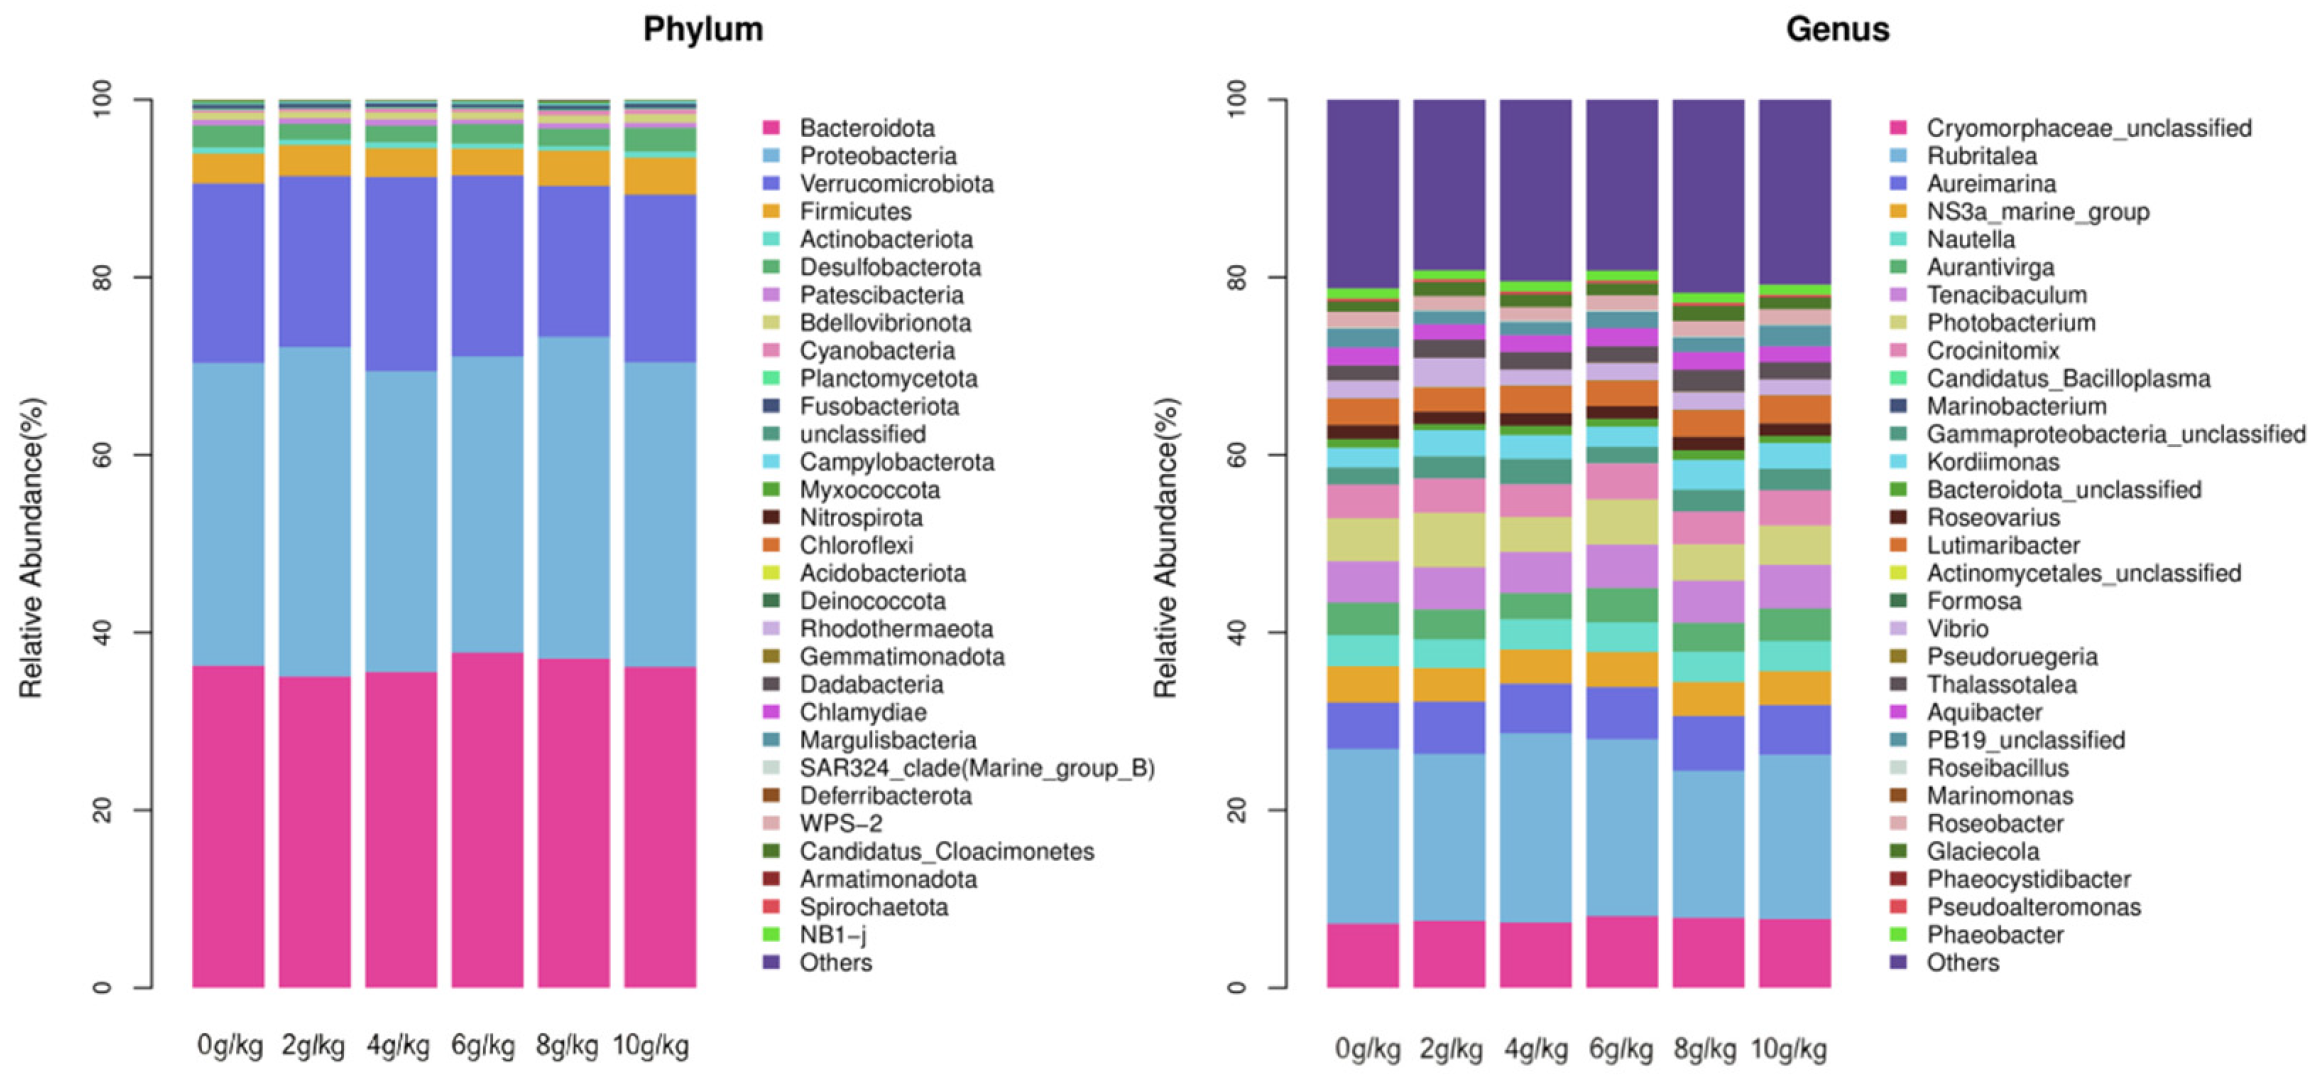
The microbial community composition in the aquaculture water at the phylum level revealed that bacterial groups with a relative abundance greater than 1% were considered core microbiota (Figure 8). The core bacterial phyla included Bacteroidota (36.31%), Proteobacteria (34.81%), Verrucomicrobiota (19.60%), Firmicutes (3.54%), and Desulfobacterota (2.16%). At the genus level, bacterial groups with a relative abundance greater than 1% were also considered core microbiota. The core bacterial genera in the aquaculture water included Rubritalea (19.12%), Cryomorphaceae (7.65%), Aureimarina (5.73%), Tenacibaculum (4.76%), and Photobacterium (4.75%).
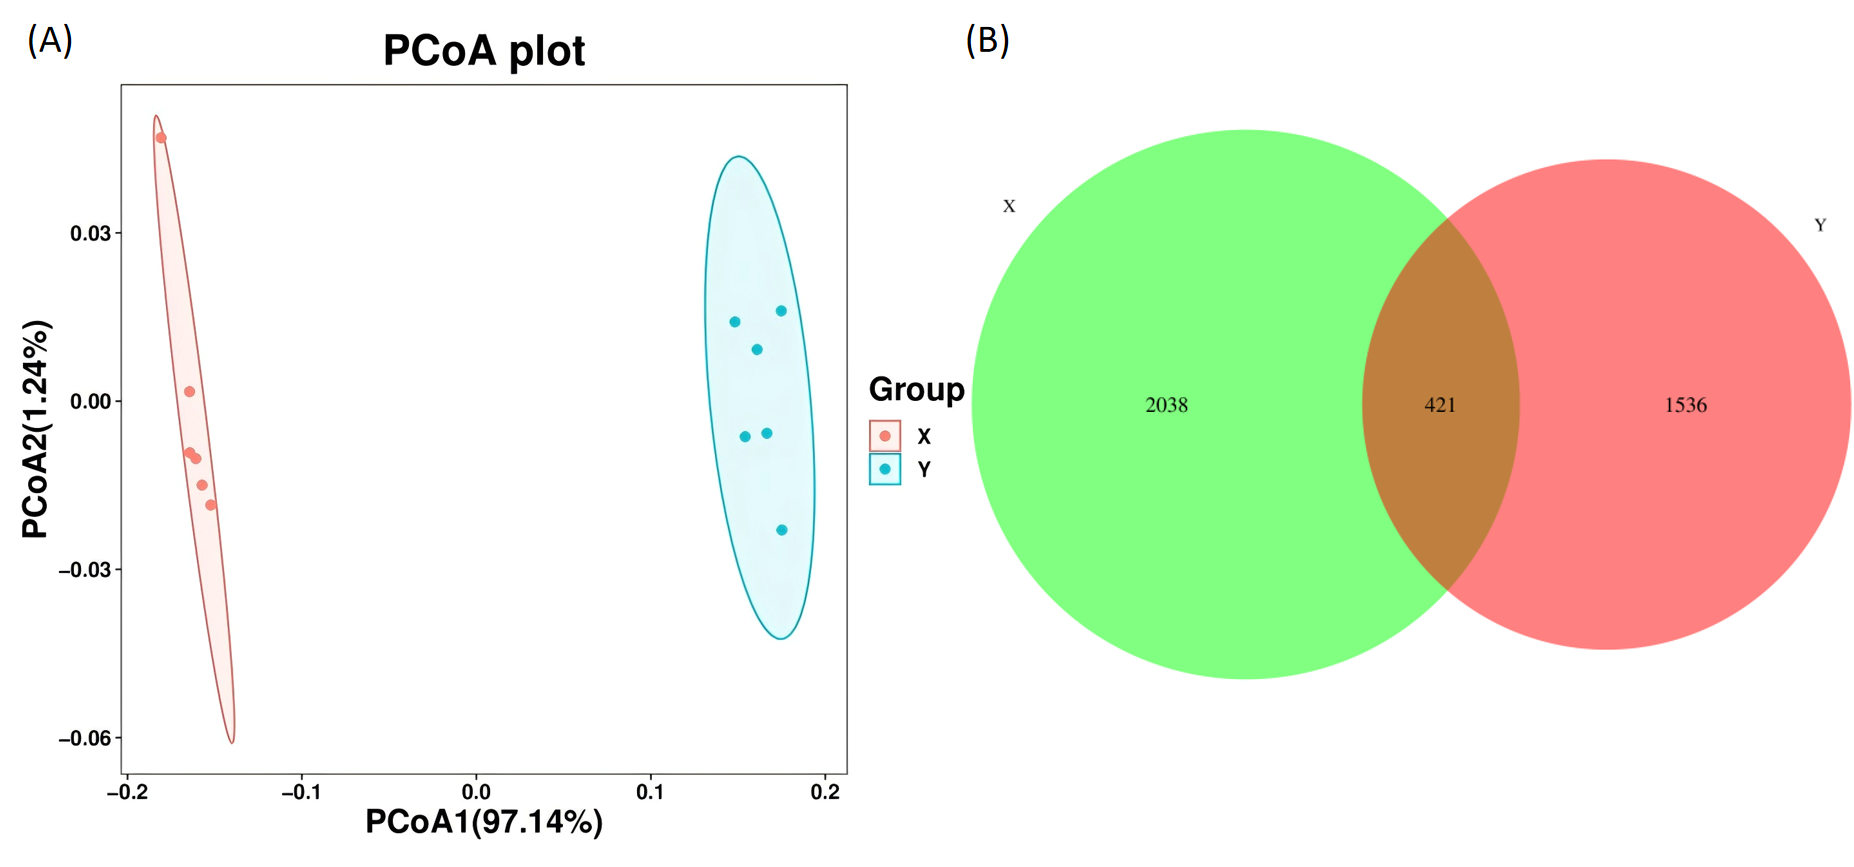
To explore the relationship between the gut microbiota of hybrid grouper and the microbial community in the aquaculture water (Table 5), a total of 2,332,076 valid sequences were obtained from 36 samples, with an average of 62,778 ± 2812 sequences per sample, ranging from 59,966 to 65,590 sequences. A comparison revealed that the number of OTUs in the gut microbiota of hybrid grouper was significantly lower than that in the aquaculture water. Specifically, the gut microbiota contained 1536 OTUs, which primarily belonged to Firmicutes and Proteobacteria, whereas the aquaculture water had 2038 OTUs, mainly classified under Proteobacteria and Bacteroidota. The two environments shared 421 OTUs in total.
As shown in Table 5, throughout the aquaculture period, the observed taxonomic units, Shannon index, species richness index, and Simpson index in the aquaculture water did not show significant changes (p > 0.05). Notably, these indices were significantly lower in the gut microbiota of hybrid grouper compared to the aquaculture water (p < 0.05).
Further analysis of bacterial communities in the aquaculture water was conducted using principal coordinate analysis (PCoA) (Figure 9). The first and second principal coordinates accounted for 97.14% and 1.24% of the total variation, respectively. The results clearly showed that samples from the same group clustered closely together, forming a distinct group. Interestingly, there was a clear separation between the gut microbiota of pearl gentian grouper and the microbial community of the aquaculture water, indicating significant differences in microbial composition between the two environments.

4. Discussion

4.1. Growth Performance, Feed Efficiency, and Survival of Fish

Known for its non-toxic and non-residual properties, GML offers various biological and nutritional benefits, including energy provision [7,14,15,16]. Research has demonstrated its positive effects on animals, for example, in improving intestinal histomorphology and enhancing feed conversion efficiency and meat quality in broilers [17,18], improving daily weight gain in finishing beef cattle [19], and improving antioxidant capacity, inflammatory response, and microbiota dysbiosis in yellow croaker [20]. These findings underline its potential to support intestinal health and overall performance in diverse species. Building on this evidence, this study investigated the impact of dietary GML on the growth and intestinal health of ♀ E. fuscoguttatus × ♂ E. lanceolatus. The findings of this study indicate that the inclusion of GML in the diet of the hybrid grouper can have a beneficial impact on its performance. The results demonstrate a dose-dependent response to GML, with clear evidence that 4 g/kg is the optimal supplementation level for maximizing growth and efficiency metrics. Despite similar IBWs across treatments, the significant increase in FBW at 4 g/kg, along with peak WG, suggests that this level provided the most favorable conditions for growth. The trend of declining FBW and WG at higher GML levels indicates a threshold beyond which supplementation becomes less effective, likely due to metabolic or physiological limitations. The CF data provide additional insights into the relationship between GML and body robustness. While CF was highest at lower GML levels (0 and 2 g/kg), the marked reduction at 10 g/kg suggests potential negative effects of excessive supplementation, thus highlighting the importance of balancing growth enhancements with body condition to ensure overall health. The positive impact of GML on weight gain has already been reported in terrestrial [16] and aquatic organisms [8,9,21]. The positive impact of GML on weight gain in animals can be attributed to its modulation of gut microbiota, enhancement of metabolic processes, and anti-inflammatory properties. GML acts as a food emulsifier that influences microbial communities, leading to improved nutrient absorption and metabolic health [22]. The mechanism also involves improved nutrient uptake due to the broadening of intestinal folds [23]. Furthermore, fatty acids are known to stimulate the metabolic rate by supporting lipid metabolism and maintaining intestinal balance by reducing triglyceride and cholesterol levels while increasing antioxidant capacity [9,24,25], which facilitates swift organismal growth and development. GML also exhibits anti-inflammatory properties, reducing systemic inflammation and promoting a healthier metabolic state, which is crucial for weight gain [5,9].
The FCR serves as a critical indicator of dietary efficiency in aquaculture, and the results demonstrate significant improvements with GML supplementation. The optimal FCR observed at 4–6 g/kg indicates efficient nutrient utilization at these levels, which likely contributes to the enhanced growth metrics. Although the increase in FCR at 8 and 10 g/kg was not statistically significant, the numerical trend is consistent with the possibility that excessive GML may impair metabolic processes, a notion supported by previous studies showing that excessive GML can alter hepatic metabolism and reduce feed efficiency in livestock [26,27].
The SGR, a complementary metric, and the SR, both peaked at 4 g/kg, aligning with the trends observed in FBW and WG. Moreover, the significant improvement in SR at this level suggests that GML may enhance the fish’s resilience to environmental or physiological stressors, potentially through its known antimicrobial and immuno- modulatory properties [16]. When feeding conditions are held constant, a marked increase in overall performance is observed. Consequently, the incorporation of GML as an additive is advocated for in the cultivation of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus and potentially other fish species to bolster economic yields.

4.2. Muscle Compositional Parameters of Fish

Regarding nutrient composition, the results showed an initial increase followed by a decline in the levels of crude fat, crude protein, and ash in muscle tissue. GML is a medium-chain fatty acid, and medium-chain fatty acids have a positive effect on improving the quality of livestock meat. The result observed in crude fat is consistent with juvenile Atlantic salmon studies [28], which suggest that MCFAs can elevate the crude fat content in muscle, whereas excess may lead to a pronounced decrease. This effect may be attributed to GML’s role in curbing lipid synthesis through the inhibition of fatty acid synthetase (FAS) and glucose-6-phosphate dehydrogenase (G6PD) activities [29]. Similarly, in hybrid grouper, GML at 1.8 g/kg (a level that closely matches 2 g/kg in the present study) increased beneficial fatty acids and reduced saturated fatty acids, potentially improving muscle quality while also enhancing antioxidant capacity, which supports overall muscle health [9].
The increase in crude protein followed by a decrease in content suggests that the proper amount of dietary GML supplementation supports protein retention, echoing the findings of previous studies [30]. Metabolic adaptations may lead to a decline in nutrient levels as the body adjusts to the new dietary composition [31]. Studies on pompano Trachinotus ovatus and hybrid grouper ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus highlight GML’s potential to enhance muscle nutritional value and biochemical composition. In pompano, GML supplementation at 1.5 g/kg significantly improved protein deposit rates and reduced triglyceride levels, reflecting enhanced protein retention and a shift toward leaner muscle composition [24]. However, higher levels of GML (above 1.5 g/kg) can still positively affect lipid metabolism and gene expression related to fat synthesis, but beyond this point, the benefits may not significantly increase. Notably, the expression of genes related to fatty acid synthesis is significantly lower in higher-GML-content diets, indicating that higher GML levels may continue to influence lipid metabolism positively. However, the specific benefits in terms of growth performance are not attained [24].

4.3. Intestinal Morphology of Fish

Measuring MLT, PW, and PH in the fish intestine is essential for evaluating the impact of dietary changes on fish growth and health. MLT indicates muscle development and nutrient utilization, while PW and PH reflect lipid metabolism and absorption efficiency [32]. These parameters correlate with growth performance metrics like weight gain and feed efficiency, aiding in optimizing feed formulations. Abnormalities in these measures can signal stress or poor nutrition, guiding adjustments in diet composition [33]. In this investigation, the introduction of GML to the diet resulted in an increased number of intestinal folds. Furthermore, dietary GML significantly increased the PH in the foregut. This positive effect is likely due to the ability of fatty acids to reduce intestinal cell necrosis by inhibiting the mRNA expression of receptor-interacting protein kinase 3 (RIP3) and mixed series protein kinase-like domains (MLKL) [34]. This finding aligns with previous research [9], which highlighted the ability of GML to increase the gut’s pH. These results suggest that incorporating dietary GML can be advantageous in improving the surface area available for intestinal nutrient absorption in the hybrid grouper. The contraction of the intestinal muscle layer is responsible for the movement of the intestines. The increase in muscle layer thickness enhances intestinal movement by pushing chyme forward. The intake of GML increased the MLT in the anterior, middle, and posterior intestines in juvenile hybrid grouper, indicating that the dietary GML supplement promotes intestinal peristalsis, facilitates nutrient absorption, and enhances the overall health and well-being of the fish.

4.4. Enzymatic and Antioxidant Activity

The results indicate that GML modulates digestive enzyme activities in hybrid grouper in a dose-dependent manner, enhancing nutrient digestion and utilization. The highest TPS activity was reached at 4 g/kg, suggesting that this level provided the most favorable conditions for protein digestion. In contrast, the 10 g/kg group showed the lowest TPS activity, indicating that the response did not increase progressively with dietary GML inclusion.
AMY activity peaked at 4 g/kg, highlighting enhanced carbohydrate digestion and energy availability at moderate GML levels. Similarly, LIP activity was highest at 4 g/kg, emphasizing the role of GML in promoting lipid digestion and energy metabolism. The enzyme responses observed at 6–10 g/kg were not superior to those at 4 g/kg, indicating that 4 g/kg was the most effective tested level for digestive enzyme activities.
Overall, GML enhances the activity of key digestive enzymes, supporting protein, carbohydrate, and lipid utilization. These findings align with improvements in growth, feed efficiency, and nutrient composition observed at 4–6 g/kg in the present study. Previous studies also reported species-dependent responses to dietary GML. In juvenile pompano (Trachinotus ovatus), GML was tested at 0–2.5 g/kg and the optimum level was estimated at 1.4–1.6 g/kg [23,24]. In white shrimp (Litopenaeus vannamei), GML was tested at 0, 0.35, 0.70, and 1.05 g/kg, with 0.70 g/kg reported as the optimal level [8]. In zebrafish (Danio rerio), dietary GML also improved intestinal lipase and protease activities [21]. These comparisons indicate that the effective dietary GML level varies among species and should be interpreted using the actual concentrations tested.
The production of free radicals and reactive oxygen species poses a significant threat to the health of aquatic animals, including fish [35,36]. To combat this, fish produce enzymatic and non-enzymatic antioxidants such as SOD, GSH, CAT, and MDA, which neutralize these harmful agents [37,38]. SOD plays a key role in eliminating free radicals and enhancing phagocytic cell activity, while MDA levels, indicative of lipid peroxidation, serve as markers of oxidative damage. GSH reduces hydrogen peroxide, contributing to immune function, and CAT protects cells from hydrogen peroxide toxicity [8,38]. Diet can significantly reduce oxidative stress in animals through the incorporation of dietary antioxidants and nutraceuticals. Research indicates that specific dietary interventions can enhance antioxidant defenses, mitigate oxidative damage, and improve overall health in various animal models. Research indicates that GML supplementation can enhance antioxidant capacity in different animal models, suggesting its potential as an effective antioxidant agent [20,39,40,41]. However, excessive fatty acid supplementation may impair the antioxidant system by triggering oxidative stress, emphasizing the need to establish a properly balanced diet for fish.
The results of this investigation also revealed a dose-dependent modulation of antioxidant activity by GML, with enhancement at 4–6 g/kg followed by a decline at 8–10 g/kg. This biphasic response indicates that antioxidant responses were most favorable within the 4–6 g/kg range, whereas increasing GML to 8–10 g/kg did not provide additional antioxidant benefits.
The peak activities CAT, MDA, and GSH in the 4 g/kg group highlight the ability of GML to enhance antioxidant defense mechanisms. CAT, a critical enzyme in neutralizing reactive oxygen species (ROS), showed significant enhancement at 4 g/kg, suggesting improved ROS detoxification. Elevated GSH levels further corroborate this, as GSH acts as a primary intracellular antioxidant that mitigates oxidative stress. The concurrent increase in MDA, a marker of lipid peroxidation, in the 4 g/kg group suggests heightened oxidative activity, likely reflecting a balance between increased ROS production due to metabolic activity and enhanced antioxidant capacity to manage it. At higher GML levels, such as 10 g/kg, the decline in CAT and GSH activities indicates that the antioxidant defense system is potentially overwhelmed. This could result from excessive ROS generation or a direct inhibitory effect of high GML concentrations on enzyme activity. The lowest GSH and CAT levels in the control and 10 g/kg groups highlight the risks of under- or over-supplementation, leading to insufficient antioxidant protection. SOD activity displayed a plateau between 6 g/kg and 8 g/kg, followed by a significant reduction at 10 g/kg. This plateau suggests a threshold effect, where moderate GML levels sufficiently support SOD activity, crucial for converting superoxide radicals into less harmful molecules. The sharp decline at 10 g/kg indicates potential oxidative stress exceeding the capacity of the SOD system, further emphasizing the limitations of excessive GML inclusion. MDA levels, indicative of lipid peroxidation, were highest in the 4 g/kg group and reduced in the 6 g/kg group, reflecting increased metabolic turnover or oxidative challenges at these levels. The intermediate MDA levels at 2, 8, and 10 g/kg, along with the lowest levels in the control group, suggest that moderate GML supplementation induces a controlled oxidative challenge that is beneficial for adaptive antioxidant responses. In contrast, the lower oxidative activity in the control and excessive GML groups could be attributed to suboptimal metabolic stimulation or compromised antioxidant capacity.
The observed trends highlight the dual role of GML in regulating oxidative activity. In the present study, 4–6 g/kg enhanced antioxidant responses, whereas responses declined at 8–10 g/kg. For comparison, a previous hybrid grouper study tested 0, 0.6, 1.2, 1.8, 2.4, 3.0, and 3.6 g/kg GML, with 1.8 g/kg identified as the optimal level for several physiological responses [9]. In juvenile pompano, dietary GML was tested at 0, 0.5, 1.0, 1.5, 2.0, and 2.5 g/kg, and 1.5 g/kg produced the highest growth-related responses, with an estimated optimum of 1.4–1.6 g/kg [24]. In white shrimp, GML was tested at 0, 0.35, 0.70, and 1.05 g/kg, and 0.35–0.70 g/kg enhanced antioxidant and antimicrobial responses [8]. Thus, the antioxidant response observed at 4–6 g/kg in the present study occurred at higher dietary inclusion levels than those reported as optimal or effective in these previous aquatic-animal studies.
GML also reduces MDA, a marker of lipid peroxidation. Significant reductions in serum MDA were observed in hybrid grouper, while hepatic MDA content decreased in pompano [9,24]. However, the effectiveness of GML in mitigating lipid peroxidation may depend on dietary composition. For example, in yellow catfish, high dietary lipid levels negated the antioxidant benefits of GML, as evidenced by elevated MDA, and reduced the expression of antioxidant-related genes such as cat, sod1, and gpx1 [32]. This suggests that the interaction between GML and dietary components like lipids warrants further investigation. In addition to its direct enzymatic effects, GML modulates oxidative stress-related gene expression. In large yellow croaker, 0.02% GML supplementation upregulated nrf2 and sod1 expression in the intestine, indicating its role in enhancing cellular antioxidant defenses [21]. Furthermore, as a medium-chain fatty acid derivative, GML provides efficient mitochondrial energy, reducing the metabolic burden on other nutrients and minimizing free radical production [24]. While not explicitly studied in this context, GML’s ability to influence gut microbiota may also contribute to improved antioxidant capacity, as beneficial microbes can enhance the host’s antioxidant system [9].
The dietary level associated with the strongest antioxidant-related responses differs among species. In the previous hybrid grouper study, 1.8 g/kg was identified as the optimal GML level [9], whereas juvenile pompano showed an optimum of 1.4–1.6 g/kg [24]. White shrimp responded to 0.35–0.70 g/kg for antioxidant and antimicrobial indices, with 0.70 g/kg reported as the overall optimal dietary level [8]. In comparison, the present study tested 0, 2, 4, 6, 8, and 10 g/kg and showed the most favorable antioxidant responses at 4–6 g/kg. These differences indicate that the effective GML level is species- and response-dependent and should be compared using actual dietary concentrations rather than qualitative terms such as “high” or “moderate”. Further research is needed to clarify the molecular mechanisms underlying these dose-dependent responses and to assess long-term effects on fish health and disease resistance.

4.5. Serum Biochemical Parameters of Fish

GML supplementation significantly influenced the serum biochemical parameters of hybrid fish in a dose-dependent manner. ALB levels increased to 4 g/kg and then declined at 6–10 g/kg. TG decreased with increasing GML up to 4–6 g/kg and showed a slight rebound at 8–10 g/kg. Similarly, CHO, HDL-C, and LDL-C declined progressively from the 2 g/kg treatment, although the magnitude of the response differed among parameters. These results indicate that the serum biochemical responses were not uniformly improved by increasing GML from 2 to 10 g/kg. The supplementation of GML and other derivatives of medium-chain fatty acids (MCFAs) and medium-chain triglycerides (MCTs) in animal diets has been shown to influence lipid metabolism [42,43].
In skeletal muscles, LDH enhances fatty acid oxidation and mitochondrial respiration, particularly in obese mice, thereby improving energy expenditure during recovery from exercise [44]. LDH also serves as a precursor for phospholipid synthesis in brain cells, indicating its importance in lipid metabolism during development [45,46]. In this investigation, LDH activity exhibited a nonlinear trend, with moderate GML doses potentially inducing adaptive metabolic shifts but higher doses impairing enzymatic function (Figure 4F). A study on the effect of GML on HD11 cells (chicken macrophage-like cell line) did not have a significant effect on the activity of LDH, thus suggesting that GML does not actively cause macrophage (a type of immune cell) activation or impact LDH activity [47].
Critical for numerous physiological processes in fish, Ca plays an important role in bone and scale mineralization, muscle contraction, blood clotting, neurotransmitter release, and osmoregulation. In laying hens’ serum, Ca concentration has been found to be significantly increased by 24.87% in a 0.30 g/kg GML group relative to the control group, indicating a positive effect of GML on Ca absorption, reflected in the enhanced eggshell strength in laying hens. Small fluctuations in calcium levels can affect skeletal integrity, neuromuscular activity, clotting efficiency, nervous system signaling, and ionic balance, especially in species under stress or living in variable salinity environments. In this study, Ca levels in the serum of hybrid fish showed a rise in the 2 g/kg treatment followed by a mild decline afterwards, hinting at altered mineral metabolism. Although a 0.5 mmol/L fluctuation may seem small, it represents a 20–25% change in calcium concentration, which is substantial for physiological systems reliant on tight calcium control. This degree of variability might suggest environmental, dietary, or metabolic stressors affecting calcium regulation mechanisms, such as gill, kidney, or intestinal function. However, in a previous study, the supplementation of GML did not influence the Ca levels in white shrimp even at relatively high concentrations up to 1.05 g/kg [8]. The possible reason why the addition of GML in the diet affects fish serum Ca is because fish rely on both diet and environmental Ca for systemic functions and GML’s potential to modulate absorption or metabolism. In contrast, shrimp’s dependence on exoskeletal calcium stores, molting cycles, and environmental calcium buffering minimize the impact of dietary GML on their serum Ca levels.
The levels of CRE and urea in fish serum play crucial roles in osmoregulation and metabolic processes. In the present study, CRE decreased across the GML treatments and remained below the control at 2–10 g/kg. Urea was also reduced across all GML treatments, although no clear dose–response pattern was observed. Therefore, the serum responses observed across the tested range of 2–10 g/kg do not support a simple linear improvement with increasing GML inclusion.

4.6. Gut Microbiota of Fish Gut and Aquaculture Water

The gut microbiota plays a crucial role in regulating digestion, nutrient absorption, and immune responses in fish, and dietary interventions can modulate its composition and functional potential [48,49,50]. In the present study, GML supplementation influenced the gut microbial structure of hybrid grouper, although principal coordinate analysis (PCoA) showed no clear separation between the control and experimental groups (Figure 5B). The stability in α diversity suggests that GML influenced microbial abundance, without inducing a drastic shift in overall community composition (Figure 6). The peak in OTUs and species richness at 6 g/kg, together with the lower OTU counts at 8 and 10 g/kg, indicates a dose-dependent response across the tested range of 0–10 g/kg. Due to its antimicrobial properties, GML is also used in aquaculture to control pathogenic bacteria [51].
Firmicutes and Proteobacteria were the dominant phyla across all groups, a common microbial profile in carnivorous fish. However, GML supplementation led to an increase in Proteobacteria abundance while reducing Firmicutes, potentially affecting gut homeostasis. Firmicutes are generally associated with fiber fermentation and short-chain fatty acid production, while Proteobacteria include both beneficial and opportunistic bacteria. The relative abundance of Vibrio, a genus that includes both commensal and pathogenic species, was notably higher in the 8 g/kg group, which also showed enrichment in genes related to the Vibrio cholerae pathogenic cycle at KEGG Level 3. This suggests that excessive GML may create conditions favorable for Vibrio proliferation, potentially increasing the risk of pathogen-associated metabolic pathways.
The LEfSe analysis further revealed that the number of distinct microbial taxa was highest in the 6 g/kg group, whereas no distinct microbial taxa were detected in the 10 g/kg group. These findings indicate that the microbial response differed across the tested dietary range of 0–10 g/kg, with 6 g/kg producing the greatest number of discriminative taxa. The KEGG functional predictions indicated that metabolism and genetic information processing were the dominant functions across all groups, with no significant differences between treatments, implying that core microbial metabolic functions were preserved despite changes in taxonomic composition.
The microbial response to GML differs among species and dietary levels. In mice, GML was tested at 0.4, 0.8, and 1.6 g/kg for 4 months, and the 1.6 g/kg treatment altered several gut microbial taxa without inducing metabolic dysfunction or systemic inflammation [22]. In juvenile pompano, dietary GML was tested at 0, 0.5, 1.0, 1.5, 2.0, and 2.5 g/kg; 1.5 g/kg produced the highest growth-related responses, with an estimated optimum of 1.4–1.6 g/kg, while the 2.0 and 2.5 g/kg treatments also altered specific bacterial taxa [23]. In a previous hybrid grouper study, GML was tested at 0, 0.6, 1.2, 1.8, 2.4, 3.0, and 3.6 g/kg, and 1.8 g/kg significantly improved several physiological and microbial responses [9]. These concentrations are all below the 2–10 g/kg range tested in the present study, emphasizing that direct dose comparisons are important when interpreting terms such as “high” or “moderate”. In addition, dietary lauric acid (LA), a hydrolysis product of GML, has been examined in swimming crab at 0.09–2.91 g/kg. The 2.91 g/kg LA treatment was associated with metabolic disorders and tissue damage, whereas microbial abundance was highest at 1.53 g/kg LA [52]. Because LA is a GML derivative rather than GML itself, these values should not be interpreted as directly equivalent to dietary GML concentrations. Overall, the present results show that microbial responses to GML are species- and dose-dependent, and comparisons should be based on the actual dietary concentrations tested.
Comparison of gut microbiota with aquaculture water microbiota revealed clear distinctions, with a significantly lower number of OTUs in fish gut microbiota. This suggests that host-associated selective pressures shape microbial composition, favoring Firmicutes and Proteobacteria over the more diverse Proteobacteria- and Bacteroidota-rich community in the surrounding water (Figure 8). The clear separation between the gut and water microbiota in PCoA analysis further supports this host-driven microbial differentiation (Figure 9). Overall, our findings suggest that dietary GML modulates gut microbiota composition in hybrid grouper across the tested range of 0–10 g/kg. While moderate levels (4–6 g/kg) appear to enhance microbial richness, higher doses may favor opportunistic bacterial taxa, including Vibrio, which could have implications for gut health. Future studies should focus on the long-term effects of GML on gut microbiota stability and host immune responses to determine optimal supplementation levels for sustainable aquaculture practices.

5. Conclusions

The results revealed the positive impact of introducing GML into the diet of hybrid groupers, demonstrating multiple benefits such as improved antioxidant activity, enhanced weight gain, and better intestinal function and health. Specifically, the present study demonstrated a nonlinear dose–response relationship between dietary GML supplementation and growth performance in hybrid grouper. Moderate GML supplementation promoted growth and feed utilization, whereas higher supplementation levels did not provide additional benefits. Based on the observed growth responses and dose–response analysis, approximately 4 g/kg GML was associated with the most favorable growth performance. The notable improvements in intestinal structure further emphasize the potential advantages of incorporating GML into grouper aquaculture practices. These findings have significant implications for the aquaculture industry, providing valuable insights that could contribute to the development of sustainable and efficient fish feed formulations.

Author Contributions

Conceptualization, S.Y.; methodology, S.Y. and L.P.; software, S.Y.; validation, F.C. and L.P.; formal analysis, S.Y. and H.E.V.; investigation, H.E.V.; data curation, D.Z. and X.W.; writing—original draft preparation, S.Y.; writing—review and editing, X.T.; supervision, D.Z.; project administration, X.T.; funding acquisition, X.T. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by the National Marine Genetic Resource Center under grant NMGRC2026NH02 and Hainan Provincial Key Laboratory of Tropical Maricultural Technologies Project under grant 2026. The authors would like to express their gratitude to the Laboratory of Environmental Physiology of Aquatic Animal for their valuable assistance during the experiment.

Institutional Review Board Statement

The animal study protocol was approved by the Institutional Review Board (Ethics Committee) of Hainan Academy of Ocean and Fisheries Sciences (protocol code EAEC-HAOFS-No.2025001, approval date: 14 April 2025).

Data Availability Statement

The data presented in this study are available in the article. Further information is available upon request from the corresponding authors.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Chen, X.X.; Ke, A.Y.; Pan, Q.C. Nutritional components analysis and nutritive value evaluation of ♀ Epinephelus fuscoguttatus× ♂ E. lanceolatus. Trans. Oceanol. Limnol. 2018, 1, 90–95. [Google Scholar] [CrossRef]
  2. Magrone, T.; Russo, M.A.; Jirillo, E. Dietary Approaches to Attain Fish Health with Special Reference to their Immune System. Curr. Pharm. Des. 2018, 24, 4921–4931. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Zorriehzahra, M.J.; Delshad, S.T.; Adel, M.; Tiwari, R.; Karthik, K.; Dhama, K.; Lazado, C.C. Probiotics as beneficial microbes in aquaculture: An update on their multiple modes of action: A review. Vet. Q. 2016, 36, 228–241. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Chen, H.; Liu, N.; He, F.; Liu, Q.; Xu, X. Specific β-glucans in chain conformations and their biological functions. Polym. J. 2022, 54, 427–453. [Google Scholar] [CrossRef] [Scilit]
  5. Mo, Q.; Fu, A.; Deng, L.; Zhao, M.; Li, Y.; Zhang, H.; Feng, F. High-dose Glycerol Monolaurate Up-Regulated Beneficial Indigenous Microbiota without Inducing Metabolic Dysfunction and Systemic Inflammation: New Insights into Its Antimicrobial Potential. Nutrients 2019, 11, 1981. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Liu, H.; Zhou, W.; Cai, C.; Feng, F.; Cai, H.; Yang, H. Biological Function of Medium-Chain Fatty Acids and Their Application in Aquatic Animals: A Review. Animals 2025, 15, 2294. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Lan, J.; Chen, G.; Cao, G.; Tang, J.; Li, Q.; Zhang, B.; Yang, C. Effects of α-glyceryl monolaurate on growth, immune function, volatile fatty acids, and gut microbiota in broiler chickens. Poult. Sci. 2021, 100, 100875. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Wang, Y.; Abdullah; Zhang, C.; Li, Y.; Zhang, H.; Wang, J.; Feng, F. Effects of dietary glycerol monolaurate on the growth performance, digestive enzymes, body composition and non-specific immune response of white shrimp (Litopenaeus vannamei). Aquac. Rep. 2020, 18, 100535. [Google Scholar] [CrossRef] [Scilit]
  9. Li, X.; Yi, Y.; Wu, J.; Yang, Q.; Tan, B.; Chi, S. Effects of Plant-Derived Glycerol Monolaurate (GML) Additive on the Antioxidant Capacity, Anti-Inflammatory Ability, Muscle Nutritional Value, and Intestinal Flora of Hybrid Grouper (Epinephelus fuscoguttatus♀ × Epinephelus lanceolatus♂). Metabolites 2022, 12, 1089. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Carvajal, O.; Nakayama, M.; Kishi, T.; Sato, M.; Ikeda, I.; Sugano, M.; Imaizumi, K. Effect of medium-chain fatty acid positional distribution in dietary triacylglycerol on lymphatic lipid transport and chylomicron composition in rats. Lipids 2000, 35, 1345–1351. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  11. Turner, N.; Hariharan, K.; TidAng, J.; Frangioudakis, G.; Beale, S.M.; Wright, L.E.; Zeng, X.Y.; Leslie, S.J.; Li, J.-Y.; Kraegen, E.W.; et al. Enhancement of muscle mitochondrial oxidative capacity and alterations in insulin action are lipid species dependent: Potent tissue-specific effects of medium-chain fatty acids. Diabetes 2009, 58, 2547–2554. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Ding, T.; Xu, N.; Liu, Y.; Du, J.; Xiang, X.; Xu, D.; Liu, Q.; Yin, Z.; Li, J.; Mai, K.; et al. Effect of dietary bile acid (BA) on the growth performance, body composition, antioxidant responses and expression of lipid metabolism-related genes of juvenile large yellow croaker (Larimichthys crocea) fed high-lipid diets. Aquaculture 2020, 518, 734768. [Google Scholar] [CrossRef] [Scilit]
  13. Fu, Z.; Zhou, S.; Yu, G.; Yang, R.; Han, M.; Ma, Z. Influence of non-protein diets on hepatic metabolism and endocrine in barramundi (Lates calcarifer). Front. Mar. Sci. 2021, 8, 649747. [Google Scholar] [CrossRef] [Scilit]
  14. Fortuoso, B.F.; Dos Reis, J.H.; Gebert, R.R.; Barreta, M.; Griss, L.G.; Casagrande, R.A.; De Cristo, T.G.; Santiani, F.; Campigotto, G.; Rampazzo, L.; et al. Glycerol monolaurate in the diet of broiler chickens replacing conventional antimicrobials: Impact on health, performance and meat quality. Microb. Pathog. 2019, 129, 161–167. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Kong, S.Z.; Li, J.C.; Li, S.D.; Liao, M.N.; Li, C.P.; Zheng, P.J.; Guo, M.H.; Tan, W.X.; Zheng, Z.H.; Hu, Z. Anti-Aging Effect of Chitosan Oligosaccharide on d-Galactose-Induced Subacute Aging in Mice. Mar. Drugs 2018, 16, 181. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  16. Kong, L.; Wang, Z.; Xiao, C.; Zhu, Q.; Song, Z. Glycerol monolaurate ameliorated intestinal barrier and immunity in broilers by regulating intestinal inflammation, antioxidant balance, and intestinal microbiota. Front Immunol. 2021, 12, 713485. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Amer, S.A.; A-Nasser, A.; Al-Khalaifah, H.S.; AlSadek, D.M.; Abdel Fattah, D.M.; Roushdy, E.M.; Sherief, W.R.; Farag, M.F.; Altohamy, D.E.; Abdel-Wareth, A.A.; et al. Effect of dietary medium-chain α-monoglycerides on the growth performance, intestinal histomorphology, amino acid digestibility, and broiler chickens’ blood biochemical parameters. Animals 2020, 11, 57. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Liu, T.; Tang, J.; Feng, F. Glycerol monolaurate improves performance, intestinal development, and muscle amino acids in yellow-feathered broilers via manipulating gut microbiota. Appl. Microbiol. Biotechnol. 2020, 104, 10279–10291. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Jordan, E.; Lovett, D.K.; Monahan, F.J.; Callan, J.; Flynn, B.; O’mara, F.P. Effect of refined coconut oil or copra meal on methane output and on intake and performance of beef heifers. J. Anim. Sci. 2006, 84, 162–170. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Tang, Y.; Zhang, Z.; Weng, M.; Shen, Y.; Lai, W.; Hao, T.; Yao, C.; Bu, X.; Du, J.; Li, Y.; et al. Glycerol monolaurate improved intestinal barrier, antioxidant capacity, inflammatory response and microbiota dysbiosis in large yellow croaker (Larimichthys crocea) fed with high soybean oil diets. Fish. Shellfish Immunol. 2023, 141, 109031. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Wang, Y.; Abdullah; Zhong, H.; Wang, J.; Feng, F. Dietary glycerol monolaurate improved the growth, activity of digestive enzymes and gut microbiota in zebrafish (Danio rerio). Aquac. Rep. 2021, 20, 100670. [Google Scholar] [CrossRef] [Scilit]
  22. Zhao, M.; Jiang, Z.; Cai, H.; Li, Y.; Mo, Q.; Deng, L.; Zhong, H.; Liu, T.; Zhang, H.; Kang, J.X.; et al. Modulation of the Gut Microbiota during High-Dose Glycerol Monolaurate-Mediated Amelioration of Obesity in Mice Fed a High-Fat Diet. mBio 2020, 11, e00190-20. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Lin, H.; Tan, B.; Yang, Q. The Effect of Glycerol Monolaurate on Intestinal Health and Disease Resistance in Cage-Farmed Juvenile Pompano Trachinotus ovatus. Aquac. Nutr. 2023, 2023, 8580240. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Lin, H.; Tan, B.; Yang, Q.; Chi, S.; Wei, H.; Wu, Y.; Ray, G.W.; Yohana, M.A. Effects of dietary glycerol monolaurate on growth, antioxidant capacity and lipid metabolism in cage-farmed pompano (Trachinotus ovatus) juveniles. Front. Mar. Sci. 2022, 9, 914134. [Google Scholar] [CrossRef] [Scilit]
  25. Xiao, S.; Jiang, S.; Qian, D.; Duan, J. Modulation of microbially derived short-chain fatty acids on intestinal homeostasis, metabolism, and neuropsychiatric disorder. Appl. Microbiol. Biotechnol. 2020, 104, 589–601. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  26. Fonseca, L.D.; Eler, J.P.; Pereira, M.A.; Rosa, A.F.; Alexandre, P.A.; Moncau, C.T.; Salvato, F.; Rosa-Fernandes, L.; Palmisano, G.; Ferraz, J.B.; et al. Liver proteomics unravel the metabolic pathways related to Feed Efficiency in beef cattle. Sci. Rep. 2019, 9, 5364. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Reyer, H.; Oster, M.; Magowan, E.; Dannenberger, D.; Ponsuksili, S.; Wimmers, K. Strategies towards Improved Feed Efficiency in Pigs Comprise Molecular Shifts in Hepatic Lipid and Carbohydrate Metabolism. Int. J. Mol. Sci. 2017, 18, 1674. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  28. Nordrum, S.; Krogdahl, Å.; Røsjø, C.; Olli, J.J.; Holm, H. Effects of methionine, cysteine and medium chain triglycerides on nutrient digestibility, absorption of amino acids along the intestinal tract and nutrient retention in Atlantic salmon (Salmo salar L.) under pair-feeding regime. Aquaculture 2000, 186, 341–360. [Google Scholar] [CrossRef] [Scilit]
  29. Clarke, S.D.; Romsos, D.R.; Leveille, G.A. Specific inhibition of hepatic fatty acid synthesis exerted by dietary linoleate and linolenate in essential fatty acid adequate rats. Lipids 1976, 11, 485–490. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Wang, Y.; Du, D.; Li, Y.; Zhang, H.; Feng, F. Effects of glycerol monolaurate on growth, health and nutritional quality of Chinese soft-shelled turtle (Pelodiscus sinensis). Chin. J. Anim. Nutr. 2019, 428–436. [Google Scholar] [CrossRef]
  31. Cassar-Malek, I.; Hocquette, J.F.; Jurie, C.; Listrat, A.; Jailler, R.; Bauchart, D.; Briand, Y.; Picard, B. Muscle-specific metabolic, histochemical and biochemical responses to a nutritionally induced discontinuous growth path. Anim. Sci. 2004, 79, 49–59. [Google Scholar] [CrossRef] [Scilit]
  32. Chen, J.; Zhuo, M.; Jiang, J.; Yu, A.; Yu, D.; Huang, F. Effects of dietary lipid levels on fiber quality, lipidomic profiles, antioxidant and inflammation responses in muscle of yellow catfish Pelteobagrus fulvidraco. Aquac. Rep. 2023, 33, 101855. [Google Scholar] [CrossRef] [Scilit]
  33. He, Y.; Liang, J.; Dong, X.; Liu, H.; Yang, Q.; Zhang, S.; Chi, S.; Tan, B. Soybean β-conglycinin and glycinin reduced growth performance and the intestinal immune defense and altered microbiome in juvenile pearl gentian groupers Epinephelus fuscoguttatus♀ × Epinephelus lanceolatus♂. Anim. Nutr. 2021, 9, 193–203. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Xu, X.; Chen, S.; Wang, H.; Tu, Z.; Wang, S.; Wang, X.; Zhu, H.; Wang, C.; Zhu, J.; Liu, Y. Medium-chain TAG improve intestinal integrity by suppressing toll-like receptor 4, nucleotide-binding oligomerisation domain proteins and necroptosis signalling in weanling piglets challenged with lipopolysaccharide. Br. J. Nutr. 2018, 119, 1019–1028. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Lushchak, V.I. Environmentally induced oxidative stress in aquatic animals. Aquat. Toxicol. 2011, 101, 13–30. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Song, C.; Sun, C.; Liu, B.; Xu, P. Oxidative Stress in Aquatic Organisms. Antioxidants 2023, 12, 1223. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Modesto, K.A.; Martinez, C.B. Effects of Roundup Transorb on fish: Hematology, antioxidant defenses and acetylcholinesterase activity. Chemosphere 2010, 81, 781–787. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Jin, M.; Lu, Y.; Yuan, Y.E.; Li, Y.I.; Qiu, H.; Sun, P.; Ma, H.-N.; Ding, L.-Y.; Zhou, Q.-C. Regulation of growth, antioxidant capacity, fatty acid profiles, hematological characteristics and expression of lipid related genes by different dietary n-3 highly unsaturated fatty acids in juvenile black seabream (Acanthopagrus schlegelii). Aquaculture 2017, 471, 55–65. [Google Scholar] [CrossRef] [Scilit]
  39. Das, R.; Sahu, N.P.; Sardar, P.; Jana, P.; Varghese, T.; Deo, A.D.; Bedekar, M.K.; Nanda, C. Glycerol monolaurate improves growth, lipid utilization and antioxidative status of white-leg shrimp, Penaeus vannamei fed with varying protein-lipid diets reared in inland saline water. Anim. Feed Sci. Technol. 2023, 306, 115794. [Google Scholar] [CrossRef] [Scilit]
  40. Famurewa, A.C.; Aja, P.M.; Maduagwuna, E.K.; Ekeleme-Egedigwe, C.A.; Ufebe, O.G.; Azubuike-Osu, S.O. Antioxidant and anti-inflammatory effects of virgin coconut oil supplementation abrogate acute chemotherapy oxidative nephrotoxicity induced by anticancer drug methotrexate in rats. Biomed. Pharmacother. 2017, 96, 905–911. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  41. Kong, L.; Cai, Y.; Pan, X.; Xiao, C.; Song, Z. Glycerol monolaurate improves intestinal morphology and antioxidant status by suppressing inflammatory responses and nuclear factor kappa-B signaling in lipopolysaccharide-exposed chicken embryos. Anim. Nutr. 2023, 15, 297–306. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  42. Shokrollahi, B.; Yavari, Z.; Kordestani, A.H. Effects of dietary medium-chain fatty acids on performance, carcass characteristics, and some serum parameters of broiler chickens. Br. Poult. Sci. 2014, 55, 662–667. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Zentek, J.; Buchheit-Renko, S.; Ferrara, F.; Vahjen, W.; Van Kessel, A.G.; Pieper, R. Nutritional and physiological role of medium-chain triglycerides and medium-chain fatty acids in piglets. Anim. Health Res. Rev. 2011, 12, 83–93. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  44. Park, S.Y.; Jung, S.R.; Kim, J.Y.; Kim, Y.W.; Sung, H.K.; Park, S.Y.; Doh, K.O.; Koh, J.H. Lactate promotes fatty acid oxidation by the tricarboxylic acid cycle and mitochondrial respiration in muscles of obese mice. Am. J. Physiol. Cell Physiol. 2024, 327, C619–C633. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Bolaños, J.P.; Medina, J.M. Lipogenesis from lactate in fetal rat brain during late gestation. Pediatr. Res. 1993, 33, 66–71. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Tabernero, A.; Bolaños, J.P.; Medina, J.M. Lipogenesis from lactate in rat neurons and astrocytes in primary culture. Biochem. J. 1993, 294, 635–638. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Kong, L.; Sun, P.; Pan, X.; Xiao, C.; Song, B.; Song, Z. Glycerol monolaurate regulates apoptosis and inflammation by suppressing lipopolysaccharide-induced ROS production and NF-κB activation in avian macrophages. Poult. Sci. 2024, 103, 103870. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  48. Gupta, S.; Vera-Ponce De León, A.; Kodama, M.; Hoetzinger, M.; Clausen, C.G.; Pless, L.; Verissimo, A.R.A.; Stengel, B.; Calabuig, V.; Kvingedal, R.; et al. The need for high-resolution gut microbiome characterization to design efficient strategies for sustainable aquaculture production. Commun. Biol. 2024, 7, 1391. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  49. Singh, B.K.; Thakur, K.; Kumari, H.; Mahajan, D.; Sharma, D.; Sharma, A.K.; Kumar, S.; Singh, B.; Pankaj, P.P.; Kumar, R. A review on comparative analysis of marine and freshwater fish gut microbiomes: Insights into environmental impact on gut microbiota. FEMS Microbiol. Ecol. 2025, 101, fiae169. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Tolas, I.; Zhou, Z.; Zhang, Z.; Teame, T.; Olsen, R.E.; Ringø, E.; Rønnestad, I. A fishy gut feeling—Current knowledge on gut microbiota in teleosts. Front. Mar. Sci. 2025, 11, 1495373. [Google Scholar] [CrossRef] [Scilit]
  51. Schlievert, P.M.; Peterson, M.L. Glycerol monolaurate antibacterial activity in broth and biofilm cultures. PLoS ONE 2012, 7, e40350. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  52. Zhan, W.; Peng, H.; Xie, S.; Deng, Y.; Zhu, T.; Cui, Y.; Cao, H.; Tang, Z.; Jin, M.; Zhou, Q. Dietary lauric acid promoted antioxidant and immune capacity by improving intestinal structure and microbial population of swimming crab (Portunus trituberculatus). Fish. Shellfish Immunol. 2024, 151, 109739. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Proximal (A), mid (B), and distal (C) intestinal histological structures of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus fed different GML (H & E × 10). MLT, muscular layer thickness; PH, plica height; PW, plica width.
Fishes 11 00519 g001
Figure 2. Effects of different dietary GML levels on the digestive enzyme activity in the intestine of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. (A) TPS activities, (B) AMY activities, and (C) LIP activities. Data are means ± SD. (n = 3). Bars with different letters represent significant differences (p < 0.05).
Fishes 11 00519 g002
Figure 3. Effects of different dietary GML levels on the enzyme activity in the intestine of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. Data are means ± SD. (n = 3). Bars with different letters represent significant differences (p < 0.05). (A) CAT, catalase; (B) ALT, alanine aminotransferase; (C) SOD, superoxide dismutase; (D) MDA, malondialdehyde; (E) GSH, glutathione.
Fishes 11 00519 g003
Figure 4. Effects of different dietary GML levels on the serum biochemical index in ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. Data are the mean ± SD. Bars with different letters represent significant differences (p < 0.05). (A) ALB, albumin; (B) TG, triglyceride; (C) CHO, total cholesterol; (D) HDL-C, high-density lipoprotein; (E) LDL-C, low-density lipoprotein; (F) LDH, lactate dehydrogenase; (G) Ca, calcium; (H) CRE, creatinine; (I) Urea.
Fishes 11 00519 g004
Figure 5. Effects of different dietary GML levels on the intestinal microbiota structure of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. (A) Venn diagram; (B) principal coordinate analysis; (C) abundance of Proteobacteria; (D) relative abundance of dominant genera.
Fishes 11 00519 g005
Figure 6. Analysis of α diversity index of intestinal microbial samples of ♀ Epinephelus fuscoguttatus × ♂E. lanceolatus under different dietary GML levels. (A) Observed OTUs; (B) Chao1 index; (C) Simpson index; (D) Shannon index. Data are the mean ± SD. Data marked with different letters were significantly different (p < 0.05) among treatments.
Fishes 11 00519 g006
Figure 7. LEfSe map of intestinal microbial difference analysis in ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. (A) 0 g/kg; (B) 2 g/kg; (C) 4 g/kg; (D) 6 g/kg; (E) 8 g/kg; (F) 10 g/kg.
Fishes 11 00519 g007
Figure 8. Microbial composition of aquaculture water with different dietary GML levels.
Fishes 11 00519 g008
Figure 9. PCoA analysis (A) and Venn diagram (B) of intestinal microorganisms of aquaculture water and the gut of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus. X denotes aquaculture water; Y denotes the fish gut.
Fishes 11 00519 g009
Table 1. Proximate composition of the experimental diets (%, dry matter percentage).
Ingredientw/%
Crude protein48
Crude lipid10
Fiber2
Ash17
Lysine4
Calcium2.5
Phosphorus1.5
Table 3. Growth performance and survival of ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus fed diets with different GML levels.
ParameterFatty Acid Levels (g/kg)
0246810
IBW (g)10.71 ± 1.5310.68 ± 1.8110.23 ± 1.789.13 ± 1.629.98 ± 1.4010.29 ± 1.62
FBW (g)170.25 ± 5.11 d182.99 ± 6.51 c221.35 ± 8.40 a199.98 ± 8.02 b195.56 ± 10.70 bc194.08 ± 6.03 bc
WG (%)1458.00 ± 81.76 d1630.79 ± 111.84 c2099.06 ± 89.06 a1848.53 ± 76.45 b1730.01 ± 127.38 bc1748.59 ± 95.76 bc
CF (g cm−3)2.06 ± 0.65 a2.11 ± 0.35 a1.81 ± 0.25 ab1.95 ± 0.17 ab1.94 ± 0.28 ab1.58 ± 0.22 b
SGR (% d−1)2.04 ± 0.11 d2.29 ± 0.13 c2.83 ± 0.14 a2.55 ± 0.12 b2.37 ± 0.19 bc2.35 ± 0.18 bc
FCR0.89 ± 0.02 a0.86 ± 0.01 b0.81 ± 0.02 c0.81 ± 0.02 c0.83 ± 0.01 c0.82 ± 0.01 c
SR (%)76.77 ± 2.67 c89.56 ± 2.33 b94.95 ± 1.01 a92.58 ± 3.54 ab92.59 ± 1.54 ab92.26 ± 1.54 ab
Note: Data are presented as mean ± SD. Data marked with different letters differed significantly (p < 0.05) among treatments. The same as below.
Table 4. Effect of the histological morphology in the intestine for ♀ Epinephelus fuscoguttatus × ♂ E. lanceolatus fed diets containing various levels of GML.
Fatty Acid Levels (g/kg)
SegmentIndex0246810
PIMLT (μm)161.37 ± 15.41 b187.78 ± 30.04 b163.42 ± 31.72 b163.75 ± 19.24 b175.60 ± 9.79 b234.32 ± 10.60 a
PH (μm)613.98 ± 48.92 bc613.98 ± 48.82 bc695.30 ± 81.43 bc654.99 ± 60.02 ab524.15 ± 60.20 c745.71 ± 19.41 a
PW (μm)67.97 ± 3.25 b64.85 ± 7.76 b91.08 ± 12.91 a64.07 ± 8.57 b74.61 ± 9.23 ab79.39 ± 9.47 ab
DIMLT (μm)155.25 ± 13.02 bc158.21 ± 20.18 bc290.72 ± 30.07 a182.00 ± 9.29 b117.32 ± 8.82 d132.07 ± 26.36 cd
PH (μm)681.25 ± 50.17 b654.49 ± 30.94 b900.39 ± 15.00 a502.24 ± 32.22 c535.47 ± 34.22 c535.25 ± 40.45 c
PW (μm)114.21 ± 18.62 a65.04 ± 6.82 bc83.07 ± 11.92 b66.47 ± 2.25 bc58.90 ± 5.34 c75.59 ± 11.36 bc
MIMLT (μm)279.52 ± 32.91 bc242.96 ± 21.69 c262.87 ± 17.33 bc336.30 ± 41.14 a313.58 ± 20.70 ab274.61 ± 18.79 bc
PH (μm)572.42 ± 59.43545.37 ± 38.19573.65 ± 57.11612.63 ± 33.76590.84 ± 39.52531.95 ± 50.70
PW (μm)93.52 ± 2.93 a76.74 ± 5.09 b64.38 ± 8.83 c63.62 ± 6.71 c77.72 ± 6.67 b55.74 ± 4.10 c
Data are presented as mean ± SD. Data marked with different letters differed significantly (p < 0.05) among treatments. Proximal (PI), distal (DI), and mid (MI) intestines; MLT, muscular layer thickness; PH, plica height; PW, plica width.
Table 5. Analysis of microbial α diversity index in aquaculture water under different dietary GML levels.
Aquaculture Water BodyObserved OtusShannonSimpsonChao1Goods CoveragePielou’s Evenness
0 g/kg858.33 ± 94.316.73 ± 1.020.97 ± 0.35858.98 ± 94.721 ± 0.000.69 ± 0.23
2 g/kg816.80 ± 39.506.96 ± 1.210.76 ± 0.20815.92 ± 38.291 ± 0.000.50 ± 0.14
4 g/kg825.19 ± 42.686.78 ± 1.150.72 ± 0.20826.87 ± 43.801 ± 0.000.49 ± 0.16
6 g/kg840.00 ± 40.206.91 ± 0.740.75 ± 0.12822.50 ± 41.001 ± 0.000.48 ± 0.08
8 g/kg880.21 ± 35.776.37 ± 1.240.76 ± 0.19821.30 ± 41.301 ± 0.000.44 ± 0.15
10 g/kg818.50 ± 41.206.03 ± 1.180.62 ± 0.23824.00 ± 42.001 ± 0.000.40 ± 0.14
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.