Article

Dissecting the Structural and Physiological Determinants of Edible Ratio and Juice Yield in a Large Lychee Germplasm Collection

Institute of Fruit Tree Research, Guangdong Academy of Agricultural Sciences, Key Laboratory of South Subtropical Fruit Biology and Genetic Resource Utilization, Ministry of Agriculture and Rural Affairs, Guangdong Provincial Key Laboratory of Tropical and Subtropical Fruit Tree Research, Guangzhou 510640, China
*
Authors to whom correspondence should be addressed.
Horticulturae 2026, 12(9), 1098; https://doi.org/10.3390/horticulturae12091098
Submission received: 30 July 2026 / Revised: 22 August 2026 / Accepted: 31 August 2026 / Published: 2 September 2026
(This article belongs to the Section Fruit Production Systems)

Abstract

Lychee (Litchi chinensis Sonn.) is a major subtropical fruit crop, yet the regulatory hierarchy underlying edible ratio (flesh weight/whole fruit weight, %) and juice yield (juice weight/whole fruit weight, %), the core processing-quality traits, remains unresolved. We phenotyped 301 accessions from ten origins under uniform conditions and used hierarchical regression to predict and evaluate edible ratio and juice yield based on structural and physiological fruit traits, thereby separating the contributions of structural constraints and physiological modulation. Both traits exhibited broad population variation and were significantly modulated by maturity stage, with late-maturing accessions outperforming early types. A strong positive correlation (r = 0.679, p < 0.001) supported the identification of “double-high” germplasm combining superior edible ratio and juice yield. Kernel ratio emerged as the dominant structural constraint on edible ratio (R2 = 0.6699, p < 0.001), while the combined inedible fraction served as the basal limiting factor for juice yield (R2 = 0.4262, p < 0.001). Critically, after controlling for structural variation, physiological traits contributed an independent 9.2% of explained variance (ΔR2 = 0.092, p < 0.001). pH was identified as the primary positive physiological predictor (β = 0.322, p < 0.001), whereas soluble solids content (SSC) exhibited a weak negative effect (β = −0.064, p = 0.008), indicating that high sugar content is not a priority target for processing-oriented breeding. An Integrated Ideotype Score (IIS) was constructed to objectively rank germplasm; elite accessions including ‘10_269’, ‘Yujinqiu’ and ‘Nuomici’ combined edible ratio > 75% with juice yield > 40%. These findings establish a “structural constraint-physiological modulation” two-tier regulatory hierarchy for lychee processing quality and provide a multivariate framework for germplasm evaluation and breeding selection.

1. Introduction

Lychee (Litchi chinensis Sonn.) is an economically important evergreen subtropical fruit tree widely cultivated in Southeast Asia. China, as the leading global producer, maintains the largest cultivation area and the highest annual output, underscoring its significance as a valuable fruit crop [1,2]. Lychee fruit quality is governed by structural and physicochemical attributes, including fruit weight, peel ratio, kernel ratio, edible ratio, soluble solids content (SSC), pH, and juice yield [3,4]. Although fresh arils remain favored by consumers for their distinctive organoleptic and nutritional qualities, recent decades have seen a marked expansion in the processing industry, yielding a diverse range of products such as clarified juices, dried arils, concentrates, and fermented beverages [5,6]. This shift in industrial demand has redirected breeding priorities from appearance-related traits suited for fresh consumption toward processing-oriented characteristics. Consequently, high edible ratio and juice yield have emerged as core agronomic targets, as they collectively influence commodity value, processing costs, and overall utilization.
To date, numerous studies have characterized phenotypic variation in fruit quality traits among commercial cultivars and clarified basic physiological regulation mechanisms of fruit development. However, these investigations have generally relied on relatively small sample sets, a limitation that undermines statistical power and prohibits robust multivariate inference [7]. By contrast, the present study evaluates 301 genetically diverse accessions, providing unprecedented statistical power for multivariate modeling of lychee processing quality. Moreover, most published studies relied on bivariate correlation analysis, which cannot distinguish direct effects from indirect confounding effects among interrelated traits [8,9]. For instance, while peel and kernel ratios are known to constrain edible flesh proportion, their independent versus mediated effects on juice yield remain unresolved because structural and physiological predictors are inherently correlated [7]. Similarly, SSC may influence juice yield through osmotic potential and cell wall pectin solubility, yet its contribution beyond structural covariation has not been quantified [5,10].
This analytical limitation is particularly critical for juice yield, which is determined by a complex interplay between structural barriers and cellular properties. Peel and kernel proportions directly limit available flesh volume, while pH-dependent pectin solubility and osmotic potential modulate juice release efficiency upon mechanical pressing [11,12]. Traditional bivariate approaches cannot partition these hierarchical contributions, fundamentally constraining the precision of trait evaluation and the effective selection of elite genotypes [13]. Hierarchical regression directly addresses this limitation by distinguishing the basal contribution of structural constraints from the incremental effects of physiological modulation, as demonstrated in apple and mango germplasm evaluation [14,15]. The ideotype concept, which integrates multiple traits into a unified selection index, enables objective ranking of genotypes with balanced performance across key attributes. However, a persistent challenge in constructing composite selection indices is the risk of overfitting when the same dataset is used to both derive model weights and rank genotypes. To mitigate this, we employed a two-step consistency-check framework: regression coefficients from the full model (M2) were used as fixed weights for the Integrated Ideotype Score (IIS), and the resulting ranking was evaluated for consistency against the K-means clustering results based on edible ratio and juice yield [16].
To overcome the constraints of small-scale studies and fill these knowledge gaps, we conducted a large-scale common-garden experiment with a total of 301 genetically diverse lychee accessions, to our knowledge, the largest germplasm panel evaluated for lychee processing quality to date. This panel comprised commercial cultivars, local landraces, and wild relatives from major production regions in southern China, providing unprecedented statistical power to dissect trait interdependencies. We employed a multi-tiered analytical framework integrating descriptive statistics, correlation matrices, collinearity diagnostics, hierarchical regression, PCA ordination, and a weighted comprehensive ideotype index. Critically, nested regression models were implemented to partition the independent contributions of structural versus physicochemical predictors to juice yield. This integrated approach establishes a trait interaction network for lychee processing quality and provides a framework for elite germplasm identification and processing-oriented breeding.

2. Materials and Methods

2.1. Plant Materials and Cultivation Management

A total of 301 lychee accessions were obtained from the National Lychee Germplasm Repository, Institute of Fruit Tree Research, Guangdong Academy of Agricultural Sciences, Guangzhou, China. Detailed information on all 301 accessions is provided in Supplementary Table S1.
Fruits were harvested at physiological maturity during the regular cropping season. All sampled trees were 15–30 years old, healthy, and free from visible pest or disease damage. Trees were maintained under standardized commercial orchard management, with uniform irrigation, fertilization, and integrated pest control across all plots. Fresh fruit samples were immediately placed in insulated foam containers for low-temperature transport, and all post-harvest processing was completed within 24 h of harvest.
All accessions were classified into four maturity groups (early, mid, late, and extra-late) based on their long-term phenological records at the National Lychee Germplasm Repository. In the Guangzhou region, the typical ripening windows for these groups are: early (before late May), mid (early June to mid-June), late (mid-June to early July), and extra-late (after early July).

2.2. Phenotypic Trait Quantification

2.2.1. Fruit Sampling

For each accession, approximately 2 kg of uniformly sized, pest-free, and mechanically undamaged mature fruits were randomly harvested from the outer canopy of each of three individual trees. Each tree served as one biological replicate. From each 2 kg batch, representative subsets of fruits were randomly selected for morphological, physicochemical, and juice yield analyses.

2.2.2. Morphological and Tissue Weight Measurement

A random subset of uniform fruits was selected from each replicate for the following measurements. Four morphology-related traits, including single fruit weight, peel weight, kernel weight and flesh weight, were quantified in this subsection. Uniform fruits from each replicate were weighed using an electronic balance (0.01 g precision) to determine single fruit weight (g). The fruit exocarp (peel) and seed (kernel) were then manually separated from the edible flesh, and the fresh weights of peel, kernel, and flesh were recorded separately.

2.2.3. Physicochemical Determinations

Two physicochemical traits, soluble solids content (SSC) and juice pH, were measured in this subsection. Juice was extracted from a randomly selected subset of fruits from each replicate. Soluble solids content (SSC, Brix) was measured from fresh juice supernatant using a digital refractometer (PAL-1, Atago Co., Ltd., Tokyo, Japan), calibrated with distilled water at 20 °C prior to use. Three technical replicates were taken per sample. Juice pH was measured at ambient temperature using a benchtop pH meter (FE28, Mettler Toledo, Greifensee, Switzerland).

2.2.4. Derived Traits

Three tissue proportion indices were calculated based on fresh tissue weights: edible ratio (%) = (flesh weight/whole fruit weight) × 100; peel ratio (%) = (peel weight/whole fruit weight) × 100; kernel ratio (%) = (kernel weight/whole fruit weight) × 100. For juice yield determination, approximately 250 g of whole fruits were randomly selected from each replicate and weighed. The fruit exocarp (peel) and seed (kernel) were then manually separated from the edible flesh, and the fresh weights of peel, kernel, and flesh were recorded separately. The flesh was pressed through sterile double-layer cheesecloth, and the resulting juice was weighed. Juice yield (%) was calculated as (juice weight/whole fruit weight) × 100.
Inedible fraction (%) was derived as the sum of the peel ratio and kernel ratio, excluding the pedicel and other non-edible tissues. Pulp juice efficiency (PJE) was calculated as juice yield/edible ratio, serving as an index of juice extraction capacity per unit of edible flesh, independent of flesh proportion variation among accessions.

2.3. Statistical Analysis

All statistical analyses were performed using R software (version 4.2.1) with the following packages: tidyverse, ggpubr, FactoMineR, factoextra, car, effectsize, patchwork, and broom. Figures were generated using ggplot2. Statistical significance was set at p < 0.05 throughout.

2.3.1. Descriptive Statistics

For each trait, mean, standard deviation (SD), coefficient of variation (CV = SD/mean × 100%), minimum, and maximum were calculated across all 301 accessions.

2.3.2. Analysis of Variance

Two-way ANOVA with origin and maturity stage as fixed factors was performed for edible ratio and juice yield. Due to unbalanced sample sizes across origin and maturity groups, Type III sums of squares were used to evaluate the unique contribution of each factor.

2.3.3. Correlation and Principal Component Analysis (PCA)

Pearson correlation coefficients were computed among all traits. PCA was performed on centered and scaled (Z-standardized) phenotypic data. Scree plots, variable loading biplots, and accession score plots (colored by origin, with 95% confidence ellipses) were generated using FactoMineR and factoextra.

2.3.4. Simple Linear Regression

Two sets of separate simple linear regression models were fitted: (1) edible ratio regressed on peel ratio and separately on kernel ratio; (2) juice yield regressed on inedible fraction, SSC, pH, and fruit weight in separate models.

2.3.5. Nested Regression and Multicollinearity Diagnostics

To partition the independent contributions of structural and physiological predictors to juice yield [15,17], a hierarchical regression approach was adopted. Two nested regression models were constructed for juice yield: M1 (structural model: juice yield ~ inedible fraction) and M2 (full model: juice yield ~ inedible fraction + SSC + pH + fruit weight). M2 was constructed by adding the three physiological predictors (SSC, pH, and fruit weight) to M1, enabling quantification of the incremental variance explained by physiological traits beyond structural constraints [15]. An additional model was fitted for PJE (PJE ~ SSC + pH + fruit weight). Standardized regression coefficients (β) were obtained from models fitted to Z-standardized data. Variance inflation factor (VIF) was calculated using the car package to diagnose multicollinearity (VIF < 5 considered acceptable [18]). The increase in R2 from M1 to M2 (ΔR2) was tested for significance using ANOVA.

2.3.6. Integrated Ideotype Score and Elite Germplasm Selection

For each accession, trait values for inedible fraction, SSC, pH, and fruit weight were standardized to Z-scores. The Integrated Ideotype Score (IIS) was calculated as the weighted sum of these Z-scores, using the standardized regression coefficients from M2 as weights. This approach follows the ideotype concept, which integrates multiple traits into a unified, regression-weighted selection index for objective genotype ranking [13,14].
Negative weights were retained to reflect the detrimental effect of the corresponding trait. All accessions were ranked by IIS, and the top 10 were selected as elite candidates.

3. Result

3.1. Germplasm Composition and Phenotypic Diversity of Quality Traits

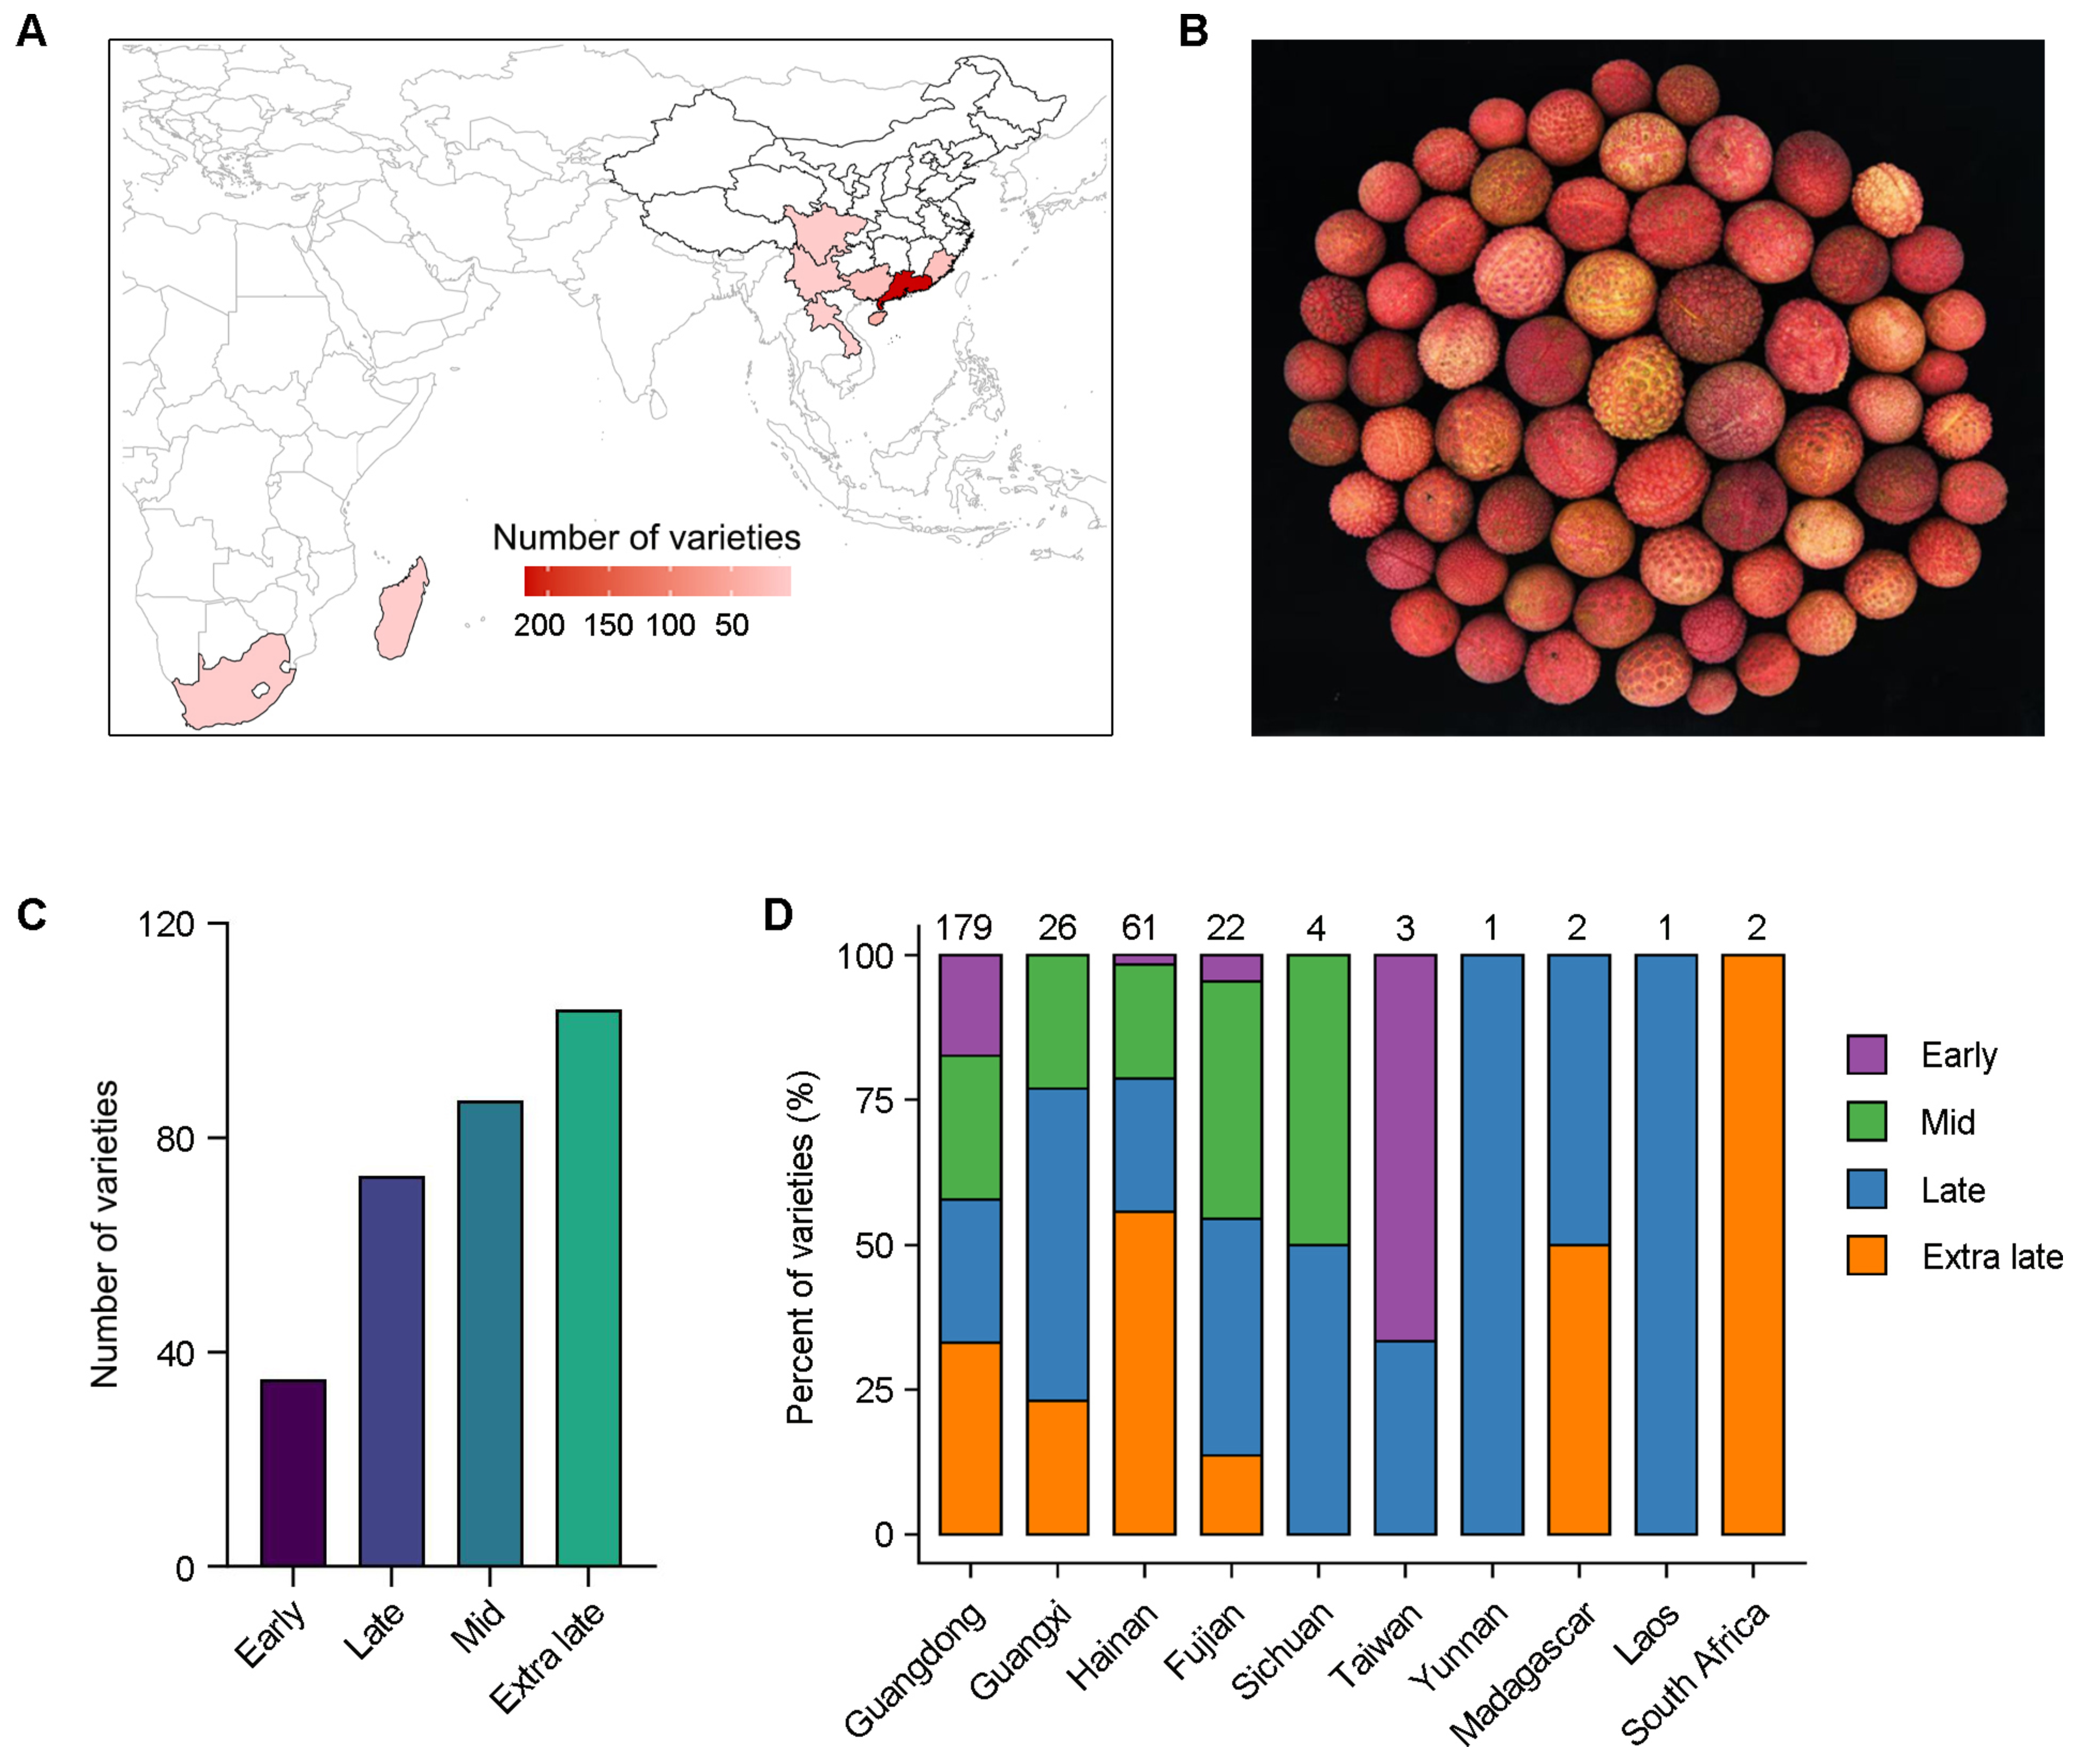
A total of 301 lychee accessions were evaluated in this study, representing ten geographic origins (Figure 1A; Table S1). Guangdong Province contributed the largest proportion of the germplasm (179 accessions, 59.47%), followed by Hainan (61 accessions, 20.27%), Guangxi (26 accessions, 8.64%), and Fujian (22 accessions, 7.31%). The remaining 13 accessions (4.32%) originated from Sichuan, Taiwan, South Africa, Madagascar, Laos, and Yunnan (Table S2). Distinct morphological diversity in fruit size and pericarp color was visible across the entire germplasm panel, as shown by representative fruit photographs (Figure 1B). In terms of maturity distribution, extra-late varieties were the most abundant (106 accessions, 35.21%), while early varieties were the least represented (35 accessions, 11.63%), indicating that the germplasm collection was dominated by mid- to late-maturing genotypes (Figure 1C,D; Table S2).
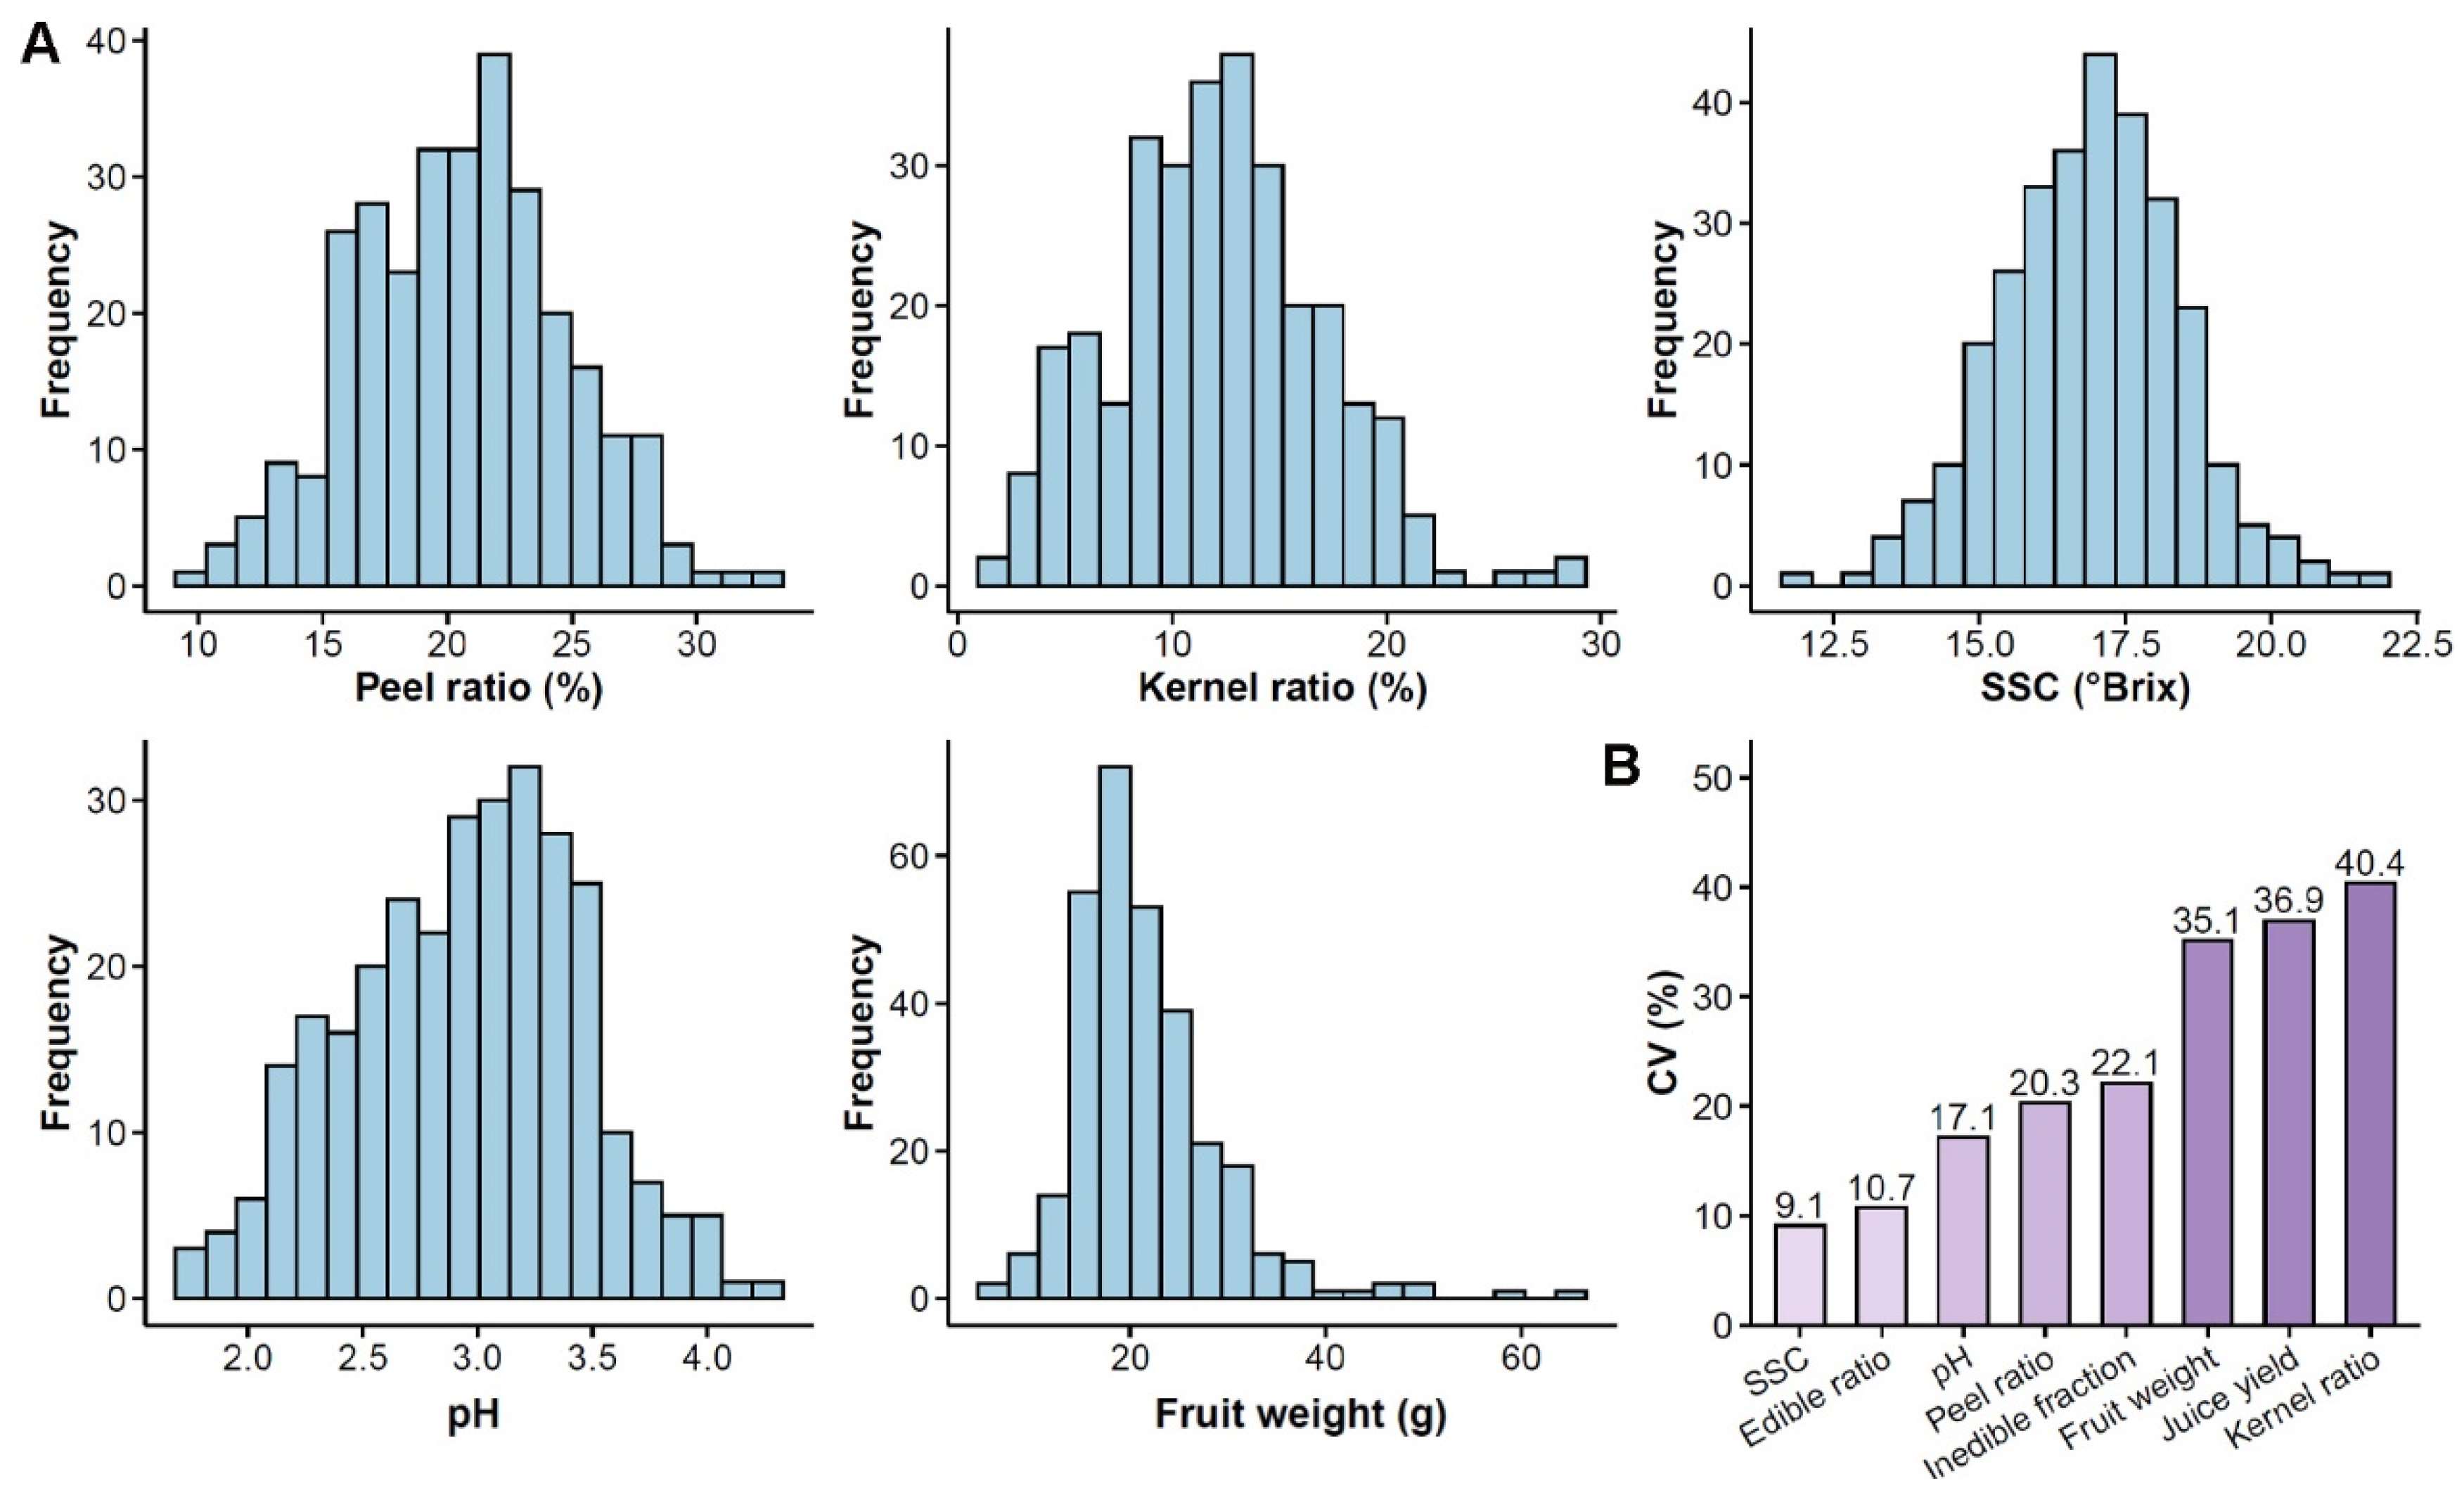
Descriptive statistics for the eight fruit quality and structural traits are summarized in Table 1, and broad phenotypic variation was observed for all measured indicators. Kernel ratio exhibited the highest coefficient of variation (CV = 40.4%), suggesting the greatest genetic diversity within the population and providing a valuable genetic basis for breeding programs targeting stenospermocarpic (chicken-tongue seed) varieties (Table 1). Juice yield (CV = 36.9%) and fruit weight (CV = 35.1%) also showed considerable variability, which offers substantial potential for genetic improvement of processing-related characteristics and fruit size (Table 1). In contrast, SSC (CV = 9.1%) and pH (CV = 17.1%) were relatively stable, suggesting that these flavor-related traits are more conserved across the germplasm collection (Table 1).
Edible ratio and juice yield also exhibited wide population variation. The mean edible ratio was 67.39% (range: 44.34–84.41%), and the mean juice yield was 30.34% (range: 8.29–56.99%) (Table 1). The substantial variation in both traits confirms the presence of elite accessions with superior combined performance within the panel.

3.2. Systematic Characterization of Edible Ratio and Juice Yield

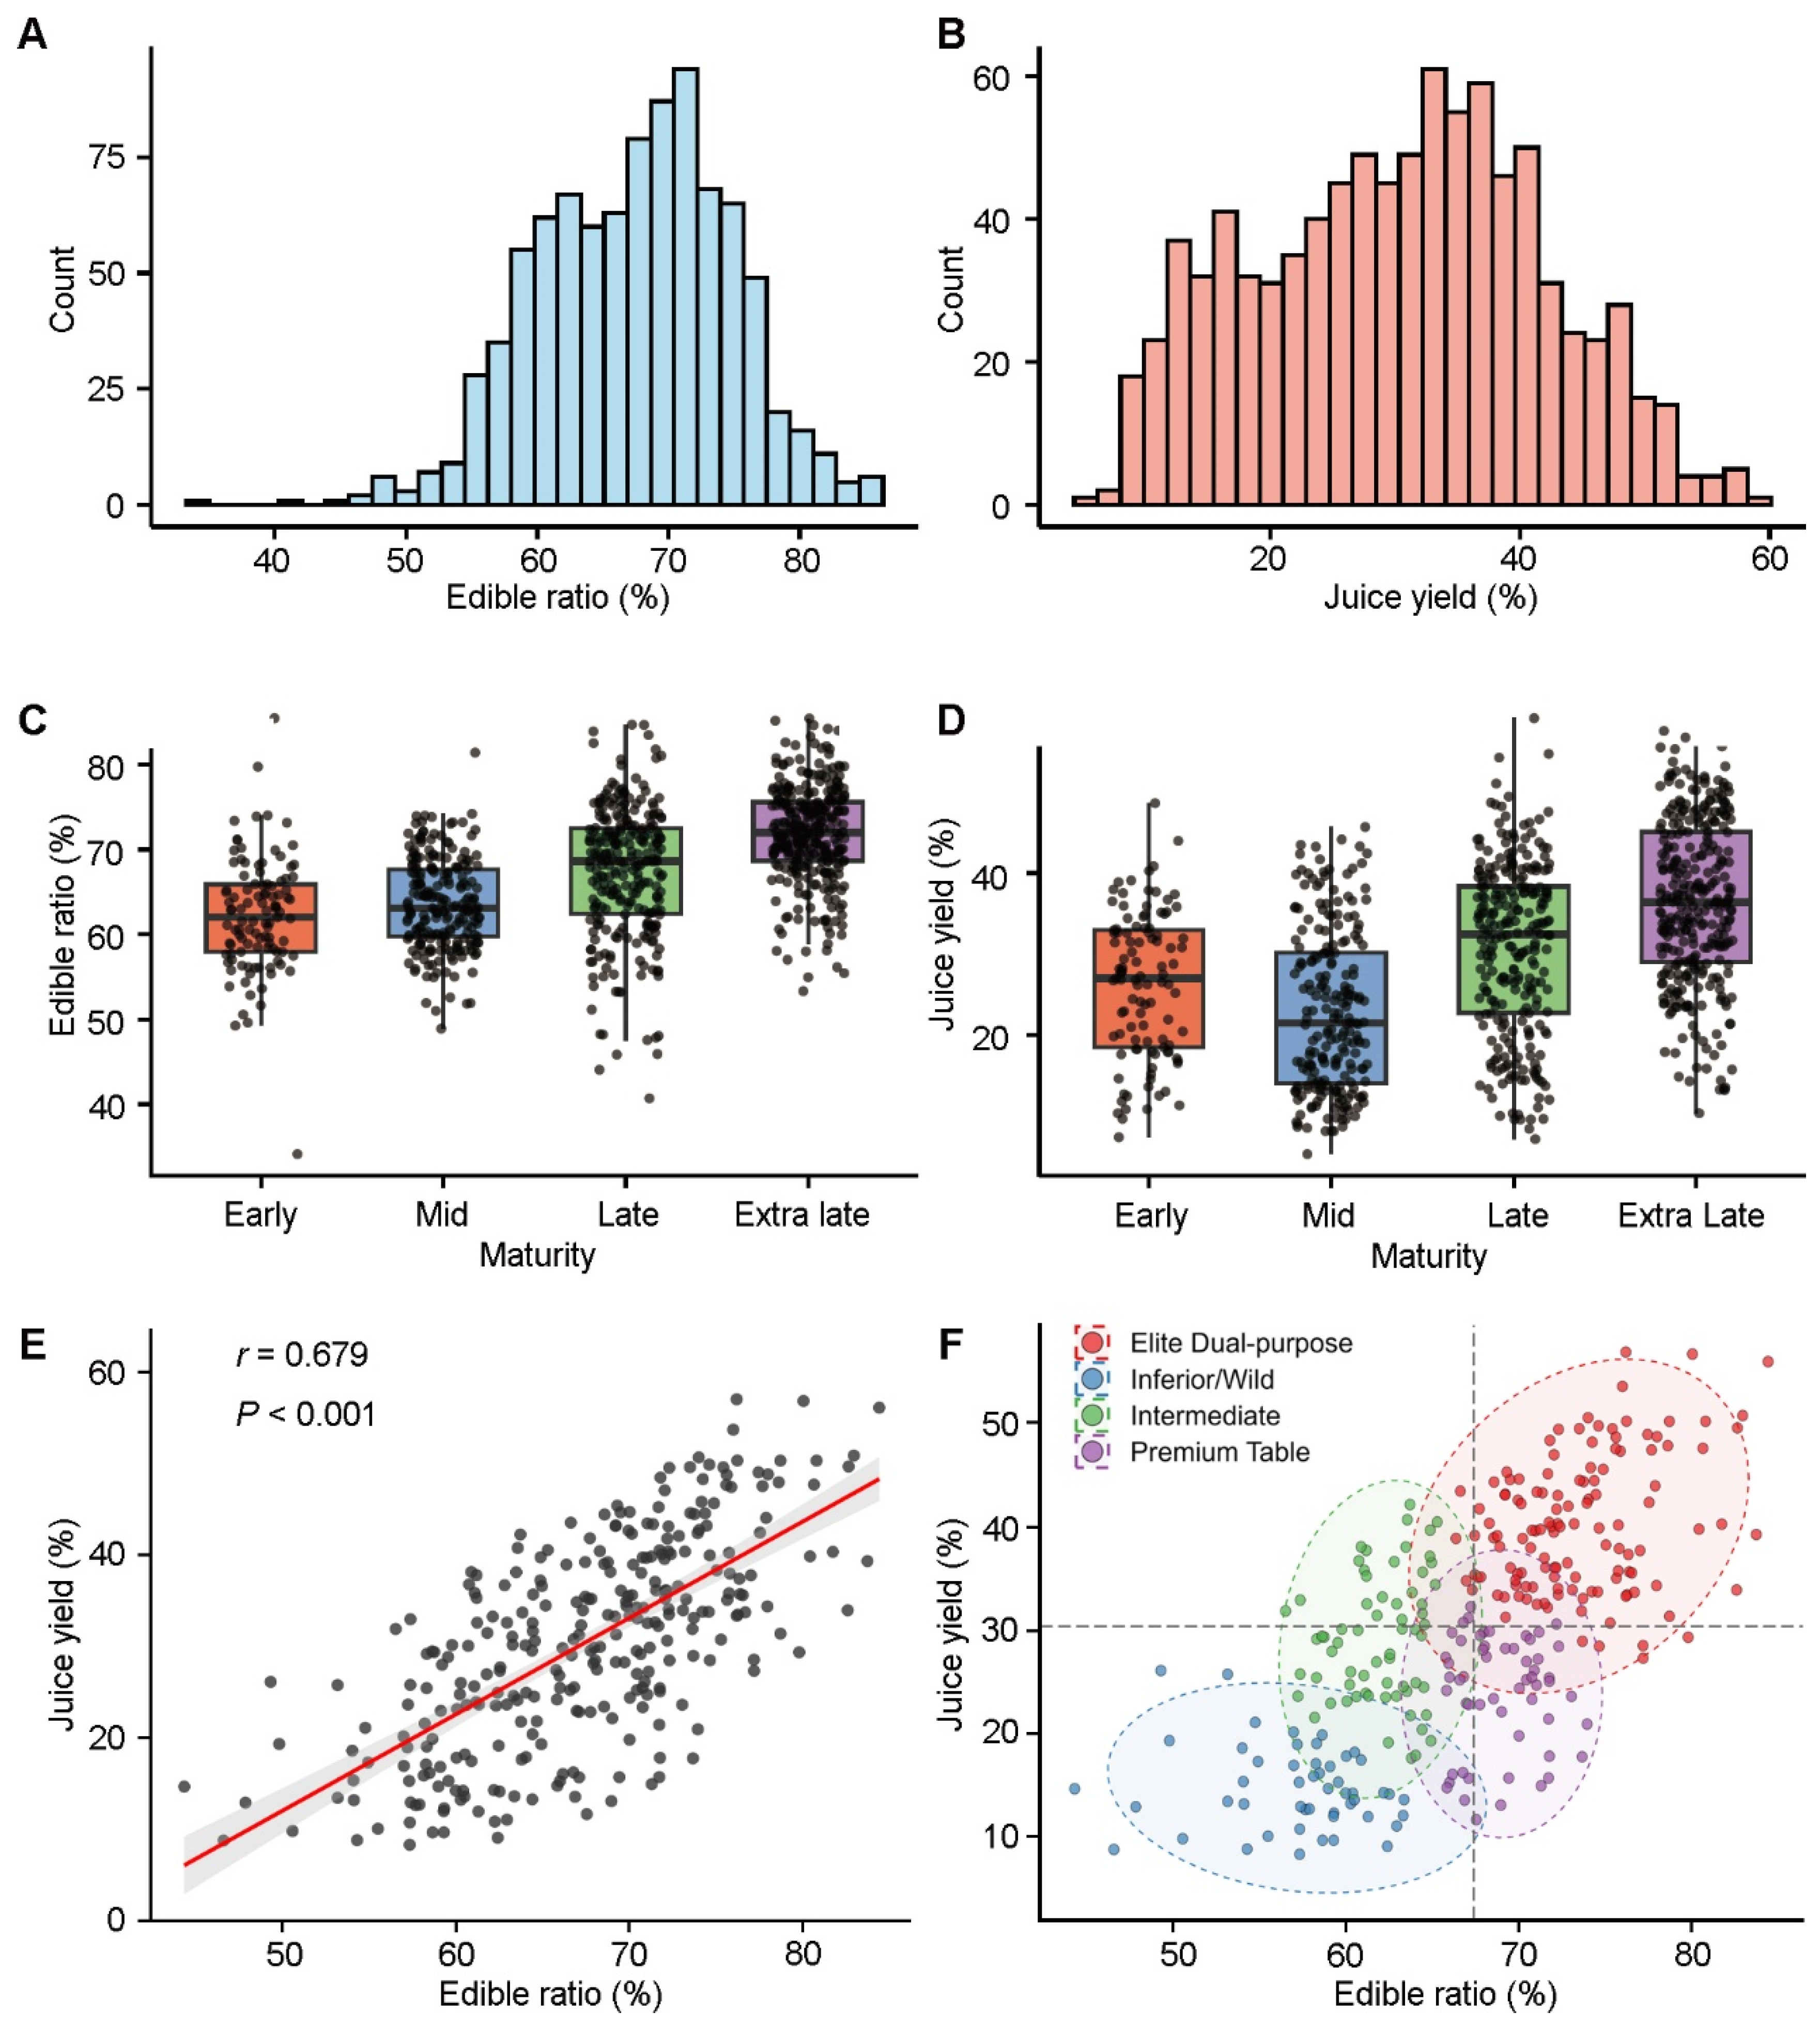
Edible ratio and juice yield were systematically characterized as the two core processing traits of lychee fruit. Both traits exhibited near-normal distributions across the population, with edible ratio concentrated between 60% and 75% and juice yield predominantly ranging from 20% to 40% (Figure 2A,B). The edible ratio distribution showed a slight right skew, indicating the presence of accessions with exceptionally high flesh proportion, while juice yield displayed a broader spread, consistent with its higher coefficient of variation (CV = 36.9%) as noted in Table 1.
Maturity stage exerted a significant influence on both traits (Figure 2C,D; Table S3). Two-way ANOVA revealed that maturity had a highly significant effect on both edible ratio and juice yield, with effect sizes substantially larger than those of origin (Table S3). Despite the smaller effect size of origin compared to maturity, substantial variation in both traits was observed across geographic origins (Figure S1). Extra-late and late-maturing accessions consistently outperformed early and mid-season types in both edible ratio and juice yield, consistent with the hypothesis that extended fruit development favors the accumulation of edible flesh and extractable juice. Correlation analysis revealed a strong positive association between edible ratio and juice yield (Pearson’s r = 0.679, p < 0.001; Figure 2E), indicating that selection for high edible ratio would indirectly improve juice yield. This moderate-to-strong correlation provided a statistical basis for the existence of elite accessions combining superior performance in both traits. To identify such elite germplasm, K-means clustering (k = 4) based on edible ratio and juice yield was applied to the lychee accessions, and the results were visualized within a four-quadrant framework (Figure 2F). The clusters were designated as Premium Table, Elite Dual-purpose, Intermediate, and Inferior/Wild according to their bivariate centroids. Dashed lines indicate the overall population means (67.7% for edible ratio and 30.7% for juice yield) and serve solely as visual references for rapid screening; they are not classification cutoffs. The upper-right quadrant, where both traits exceed the population means, was primarily occupied by the Elite Dual-purpose cluster, identifying this group as the principal source of genotypes combining superior fresh-eating and processing quality.

3.3. Phenotypic Variation in Structural and Physiological Traits

Beyond edible ratio and juice yield, the remaining five traits exhibited distinct distribution patterns (Figure 3A). Peel ratio and kernel ratio both approximated normal distributions, with means of 20.53% and 12.08%, respectively. SSC and pH also followed near-normal patterns, concentrating at 16–18 °Brix and 2.5–3.5, respectively. Fruit weight displayed right skewness, indicating that most accessions bore small fruits with few large-fruit outliers (Figure 3A). Trait variability diverged widely across the panel, with kernel ratio showing the highest CV (40.4%) and SSC the lowest (9.1%) (Figure 3B; Table 1).

3.4. Trait Correlations and Population Structure

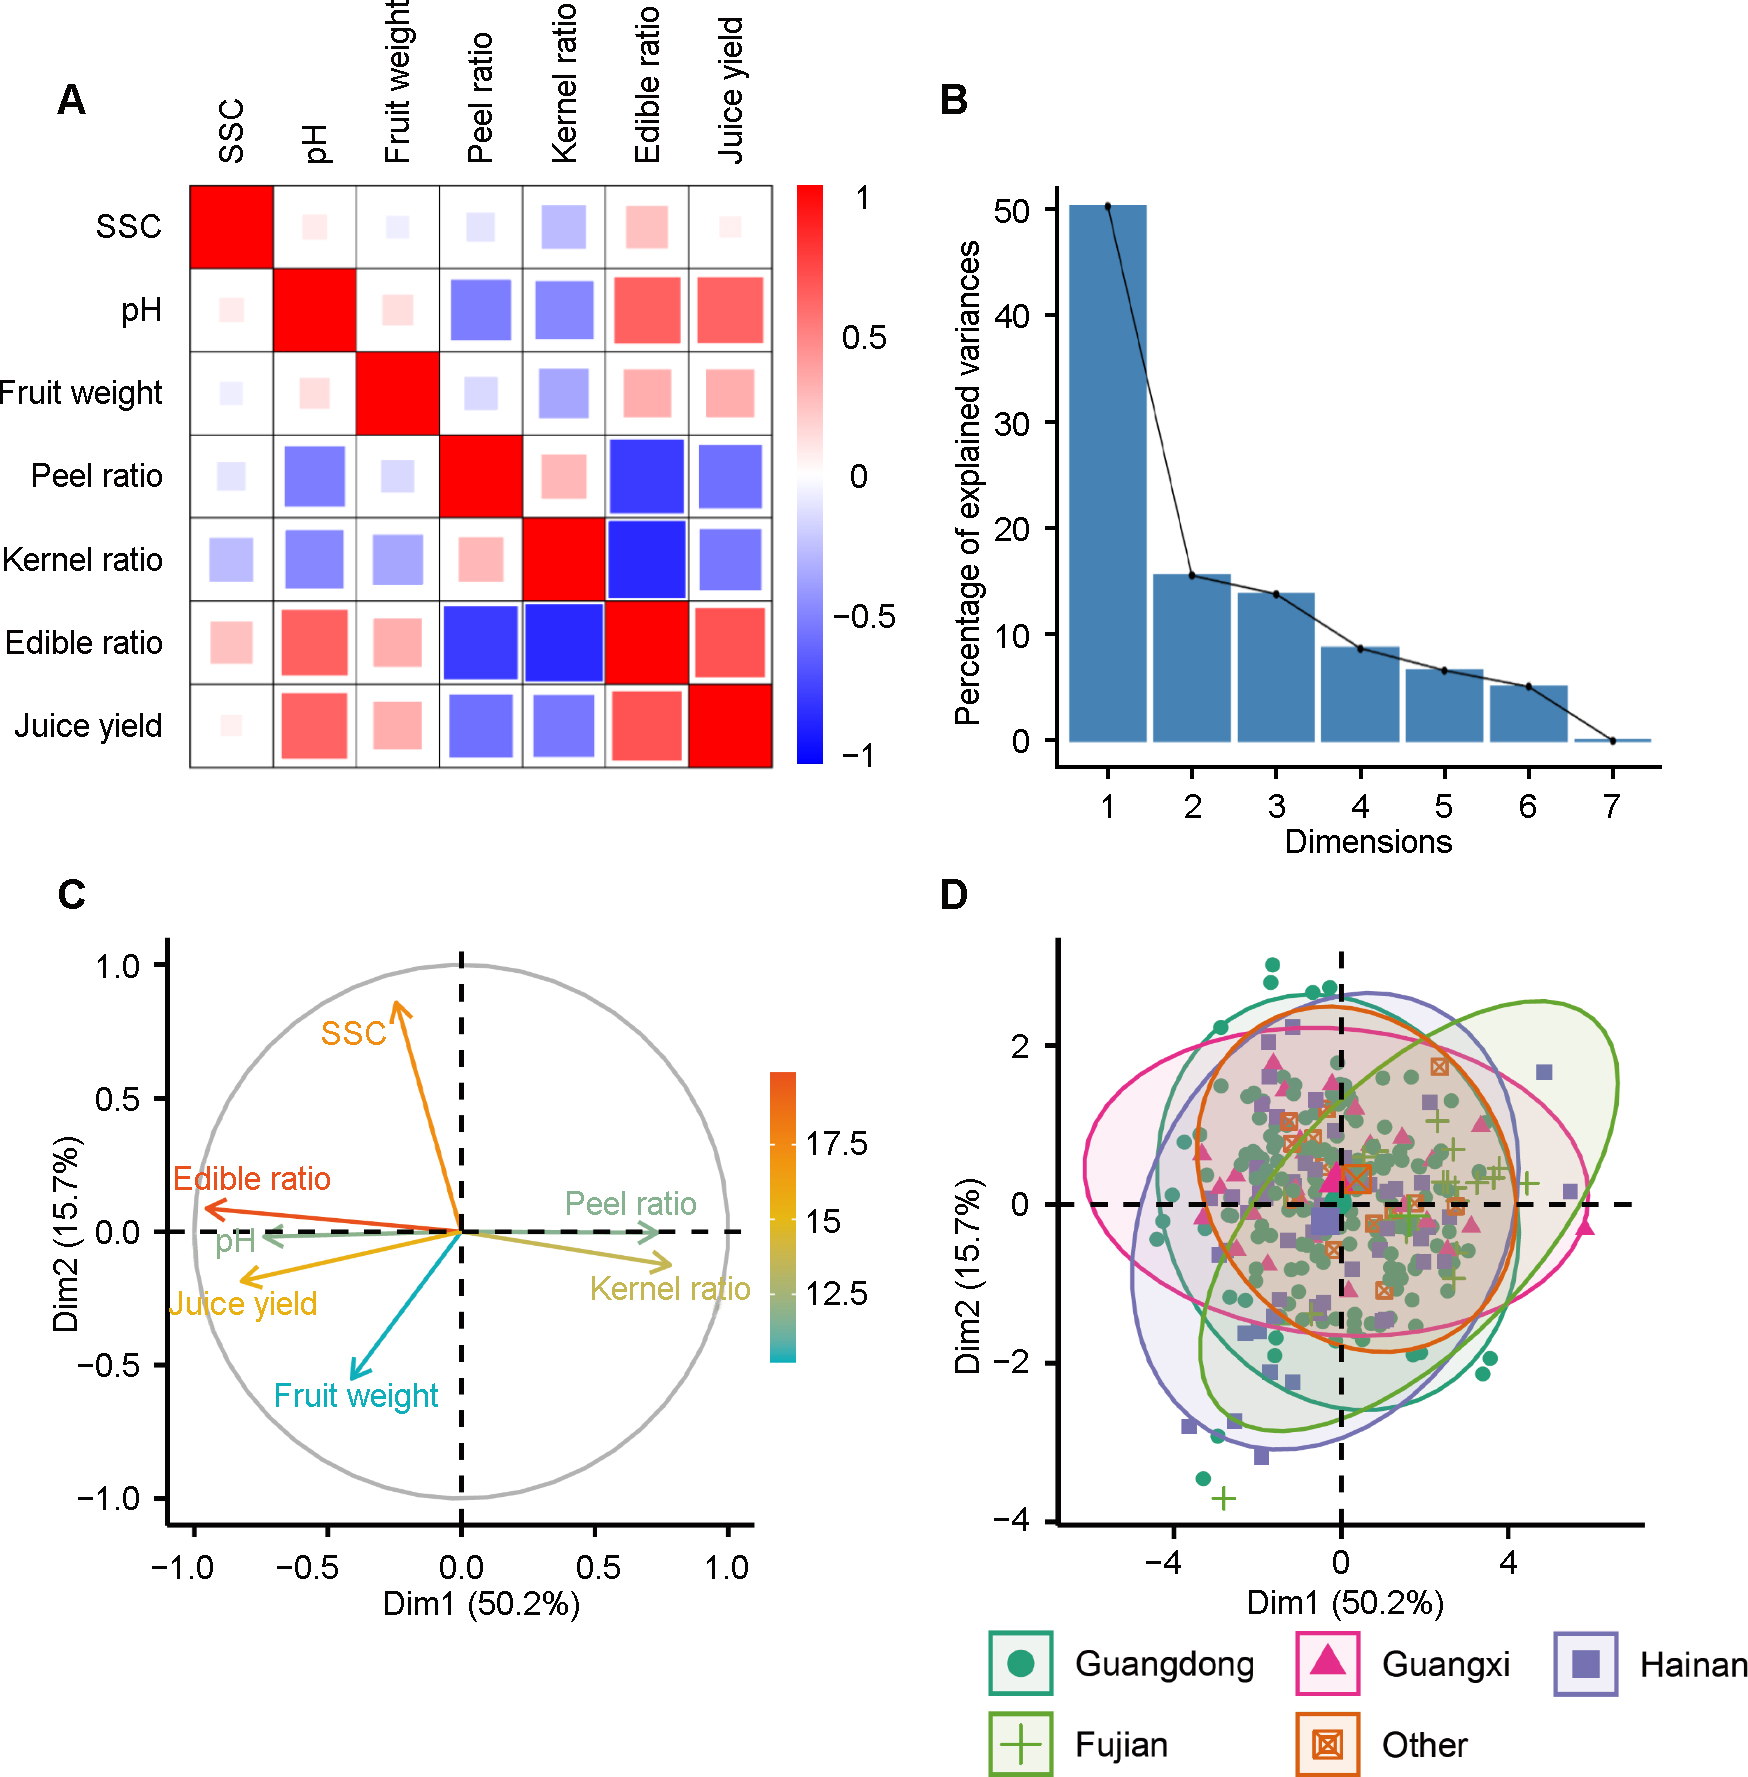
Pairwise correlations revealed strong negative associations between structural tissue proportions and edible ratio: peel ratio (r = −0.758, p < 0.001) and kernel ratio (r = −0.818, p < 0.001) were the primary constraints on flesh percentage (Figure 4A; Table S4). SSC showed no significant bivariate correlation with juice yield (r = 0.062, p = 0.298), consistent with its role as a flavor-related trait rather than a direct determinant of juice extraction. By contrast, fruit weight exhibited a significant positive association with juice yield (r = 0.321, p < 0.001). A network visualization of these correlations further highlights the modular structure of trait relationships, with structural traits forming a tightly interconnected cluster distinct from the physiological-size module (Figure S2).
PCA resolved multi-trait population stratification along two major axes (Figure 4B; Table S5a). PC1 and PC2 (Dim1 and Dim2 in Figure 4C,D) explained 50.2% and 15.7% of total variance, respectively, capturing 65.8% cumulatively. PC1 represented a structural dimension, with peel ratio and kernel ratio loading positively and edible ratio negatively along this axis (Figure 4C; Table S5b). PC2 represented a physiological-size dimension, driven by SSC (positive) and fruit weight (negative) along the second axis. The score biplot revealed geographic differentiation: Guangdong and Guangxi germplasm clustered towards higher edible ratio (negative PC1), whereas Hainan accessions scattered along PC2, reflecting their broader diversity in soluble solids (Figure 4D). All VIFs were below 2, confirming the absence of multicollinearity among predictors (Table S6).

3.5. Univariate Linear Regression Analyses of Edible Ratio and Juice Yield

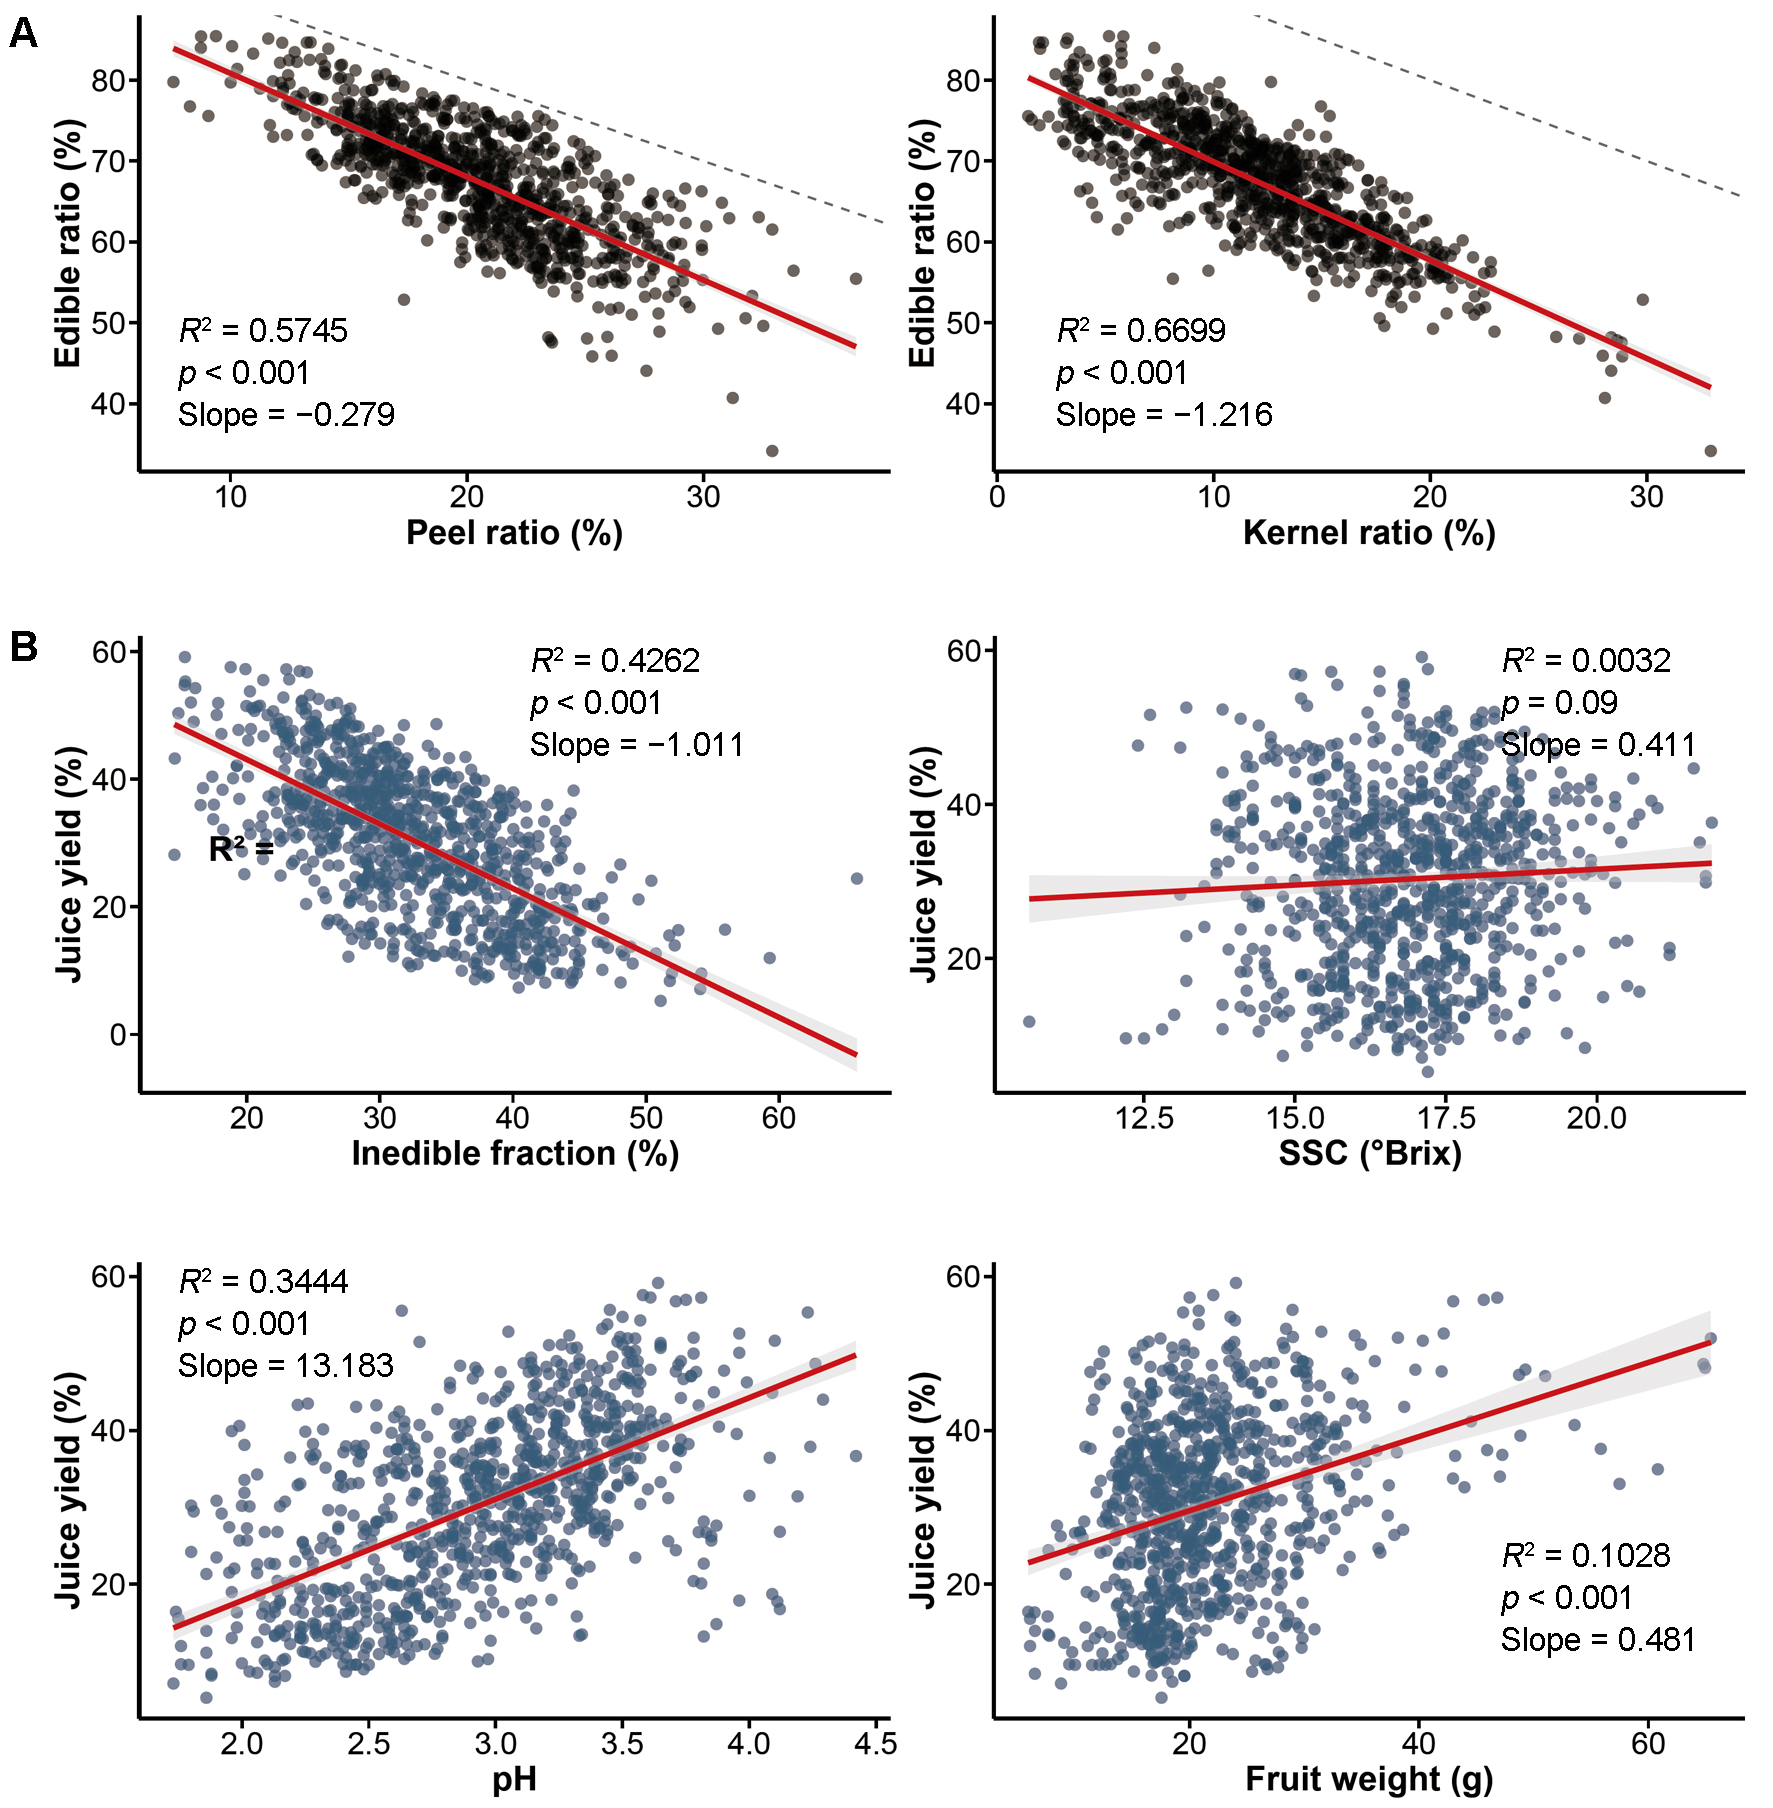
To quantify the independent linear contributions of individual traits to edible ratio and juice yield, univariate linear regression models were fitted (Figure 5). For edible ratio (Figure 5A), both peel ratio and kernel ratio showed highly significant negative associations. Peel ratio explained 57.45% of the phenotypic variation. Kernel ratio exhibited higher explanatory power, accounting for 66.99%, indicating that kernel ratio is the dominant structural constraint on edible flesh proportion.
For juice yield (Figure 5B), the total inedible fraction showed a highly significant negative correlation, explaining 42.62% of the variation in juice yield with a slope of −1.011, confirming that the combined proportion of peel and kernel is the core structural factor limiting juice yield. pH exhibited a highly significant positive correlation with juice yield, explaining 34.44% of the variation with a slope of 13.183. Fruit weight also showed a highly significant positive linear effect on juice yield, explaining 10.28% of the variation. Notably, SSC was not significantly associated with juice yield (R2 = 0.0032, p = 0.09), indicating that soluble sugar content does not independently predict juice extraction in simple linear models. Residual diagnostics (Figure S3) confirmed that assumptions of homoscedasticity and normality were satisfied for all models. These univariate results provided a foundation for hierarchical regression to disentangle the direct and indirect effects of structural versus physiological predictors.

3.6. Structural Dominance and Physiological Supplementation in Determining Juice Yield

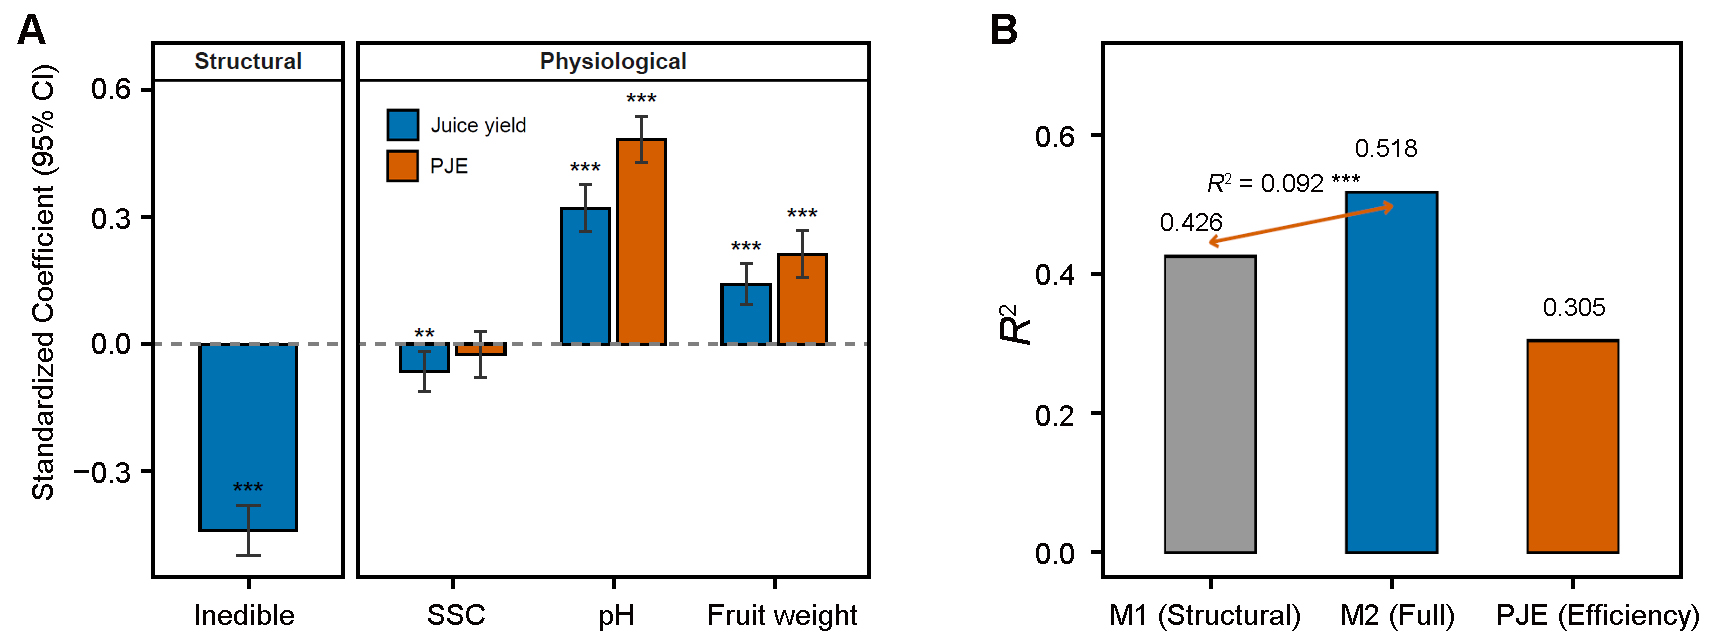
To partition the independent contributions of structural and physiological predictors on juice yield, and to test whether physiological traits contribute independently beyond structural constraints, a hierarchical regression approach was adopted. Three nested models were constructed (Figure 6A). M1, the structural model, included only the inedible fraction. M2, the full model, added SSC, pH, and fruit weight to M1. An additional model was fitted for pulp juice efficiency (PJE = juice yield/edible ratio) with SSC, pH, and fruit weight as predictors, to evaluate the physiological determinants of juice extraction per unit of flesh. Standardized regression coefficients (β) were obtained from models fitted to Z-standardized data (Table S7; Figure 6A).
In the full model (M2), the inedible fraction exhibited the strongest negative effect (β = −0.441, p < 0.001), supporting structural waste as the primary limiting factor for juice yield. pH showed a strong positive effect (β = 0.322, p < 0.001), while SSC exhibited a weak negative coefficient (β = −0.064, p = 0.008) and fruit weight a modest positive one (β = 0.141, p < 0.001). Notably, SSC was not significant in univariate regression (R2 = 0.0032, p = 0.09) but became significant after controlling for inedible fraction in M2, indicating that its effect was masked by structural variation.
The R2 values of the three models are compared in Figure 6B. M1 explained 42.6% of the variance in juice yield, while M2 raised the explained variance to 51.8%, yielding a significant ΔR2 of 0.092 (p < 0.001). This 9.2% increment demonstrates that physiological traits contribute independently to juice yield beyond structural constraints. The PJE model achieved an R2 of 0.305, indicating that pH and fruit weight together explain approximately 30.5% of the variation in flesh-specific juice extraction efficiency.
In the PJE model (Table S7; Figure 6A), pH emerged as the dominant positive predictor (β = 0.484, p < 0.001), followed by fruit weight (β = 0.213, p < 0.001); SSC was not significant (β = −0.025, p = 0.372). These contrasting results between M2 and PJE support the conclusion that pH primarily enhances juice extraction efficiency per unit of edible flesh, rather than simply elevating absolute juice yield.

3.7. Integrated Ideotype Score and Elite Germplasm Recommendation

To integrate structural and physiological determinants into a unified selection framework, an Integrated Ideotype Score (IIS) was constructed as the weighted sum of Z-standardized values for inedible fraction, SSC, pH, and fruit weight, using M2 standardized coefficients as weights (Table S7; Figure 6A). Negative weights were assigned to detrimental traits to penalize their adverse effects.
Across all accessions, IIS ranged from −2.38 to 1.67 (Figure S4A). The top five accessions are listed in Table 2. Genotype 10_269 (a hybrid progeny) achieved the highest IIS (1.67), driven by high edible ratio (82.64%) and favorable SSC (18.27 °Brix). Yujinqiu ranked second (1.58), with comparable edible ratio (82.94%), and high juice yield (50.84%). Nuomici ranked fifth (1.52); despite having the highest edible ratio (84.41%) and high juice yield (56.07%), its small fruit weight (23.85 g) reduced its composite score.
The IIS ranking was consistent with the K-means clustering results, with all top five accessions belonging to the Elite Dual-purpose cluster. IIS additionally uncovered trait trade-offs. Genotypes with superior edible ratio could not secure top composite scores if they carried suboptimal fruit weight or pH. Full IIS distribution and the top 10 accessions are shown in Figure S4. The IIS provides more balanced multi-trait evaluation for elite germplasm than screening based on only one or two traits.

4. Discussion

Edible ratio and juice yield are core traits determining the fresh-market quality and processing efficiency of fruit crops [19,20]. For lychee, however, most existing studies have been confined to small sample sets, limiting statistical power and multivariate inference [7]. This study phenotyped 301 accessions and applied hierarchical regression to disentangle structural and physiological effects on these traits.
The panel size (n = 301) exceeds typical lychee studies by an order of magnitude, providing adequate power for multivariate models [21]. Kernel ratio was the dominant structural constraint on edible ratio (R2 = 0.6699), exceeding peel ratio (R2 = 0.5745). This aligns with stenospermocarpy breeding strategies in horticultural crops, where seed abortion after fertilization allows expanded fruit development without compromising fruit size [22,23], though whether the same hormonal and transcriptional networks operate in lychee requires further study. The high CV of kernel ratio (40.4%) suggests substantial genetic variation for selection, but the edible ratio ceiling (~84%) observed even in near-stenospermocarpic accessions implies that peel ratio imposes a secondary constraint that may require simultaneous selection for thinner pericarp.
For juice yield, the inedible fraction explained 42.62% of the variation as a basal structural limit, consistent with the inverse relationship between peel thickness and juice percentage documented in citrus rootstock trials [24]. After controlling for structure, physiological traits added 9.2% explained variance (ΔR2 = 0.092). pH was the strongest physiological predictor (β = 0.322), possibly reflecting pH-dependent modulation of cell wall pectin solubility, as suggested by the central role of pectin depolymerization and middle lamella dissolution in fruit softening [25,26,27].
SSC showed a weak negative effect in the full model (β = −0.064, p = 0.008) after being non-significant in univariate regression. This small effect may reflect covariance with unmeasured structural traits or viscosity effects on juice flow, as reviewed in lychee postharvest physiology [28]; rather than interpreting SSC as a meaningful target for juice yield improvement, we suggest that breeding for high SSC would not compromise juice yield, but neither would it improve it directly. The PJE model (R2 = 0.305), where pH remained significant (β = 0.484) while SSC did not (β = −0.025, p = 0.372), suggests pH may enhance extraction efficiency per unit flesh, though this mechanism requires experimental validation.
The Integrated Ideotype Score (IIS) provided objective multi-trait ranking; top accessions (e.g., ‘10_269’) were corroborated by the Elite Dual-purpose cluster assignment from K-means analysis, although this represents an internal consistency check rather than independent validation. IIS weights derived from the same dataset may inflate apparent precision; future work should incorporate cross-validation to strengthen the generalizability of the ranking [16]. Maturity stage significantly affected both traits, with late-maturing accessions outperforming early types, consistent with extended developmental time for flesh accumulation, though causal mechanisms remain speculative. This pattern aligns with the non-climacteric nature of lychee, where fruit must ripen fully on the tree and maximum growth occurs during the final six weeks of development [29,30,31].
Several methodological considerations warrant mention. The phenotypic data were collected from a single location in a single season; while this design ensured uniform environmental conditions and minimized confounding noise, it also means that genotype-by-environment interactions were not assessable. Multi-site, multi-year evaluations would be a logical next step to test the stability of the observed trait hierarchies [32]. Regarding processing simulation, the manual cheesecloth pressing employed here reflects small-scale juice extraction. Similarly, while the IIS was based on seven processing-related traits, our germplasm evaluation only focused on fruit-level characteristics, and tree-level agronomic metrics such as per-tree yield were not recorded for this large panel of 301 accessions. Tree-level yield should be incorporated in future work to build more comprehensive selection indices for lychee breeding. Beyond that, additional attributes such as color stability, aroma retention, and browning susceptibility could be considered for inclusion in future refined selection indices. Lastly, the regression framework quantifies predictive associations rather than causal pathways; we therefore regard the pH-juice yield relationship as a testable hypothesis that awaits biochemical and genetic dissection.
In conclusion, this study proposes a preliminary two-tier regulatory framework for lychee juice yield: basal structural constraints dominate, with modest supplementary effects of physiological traits, particularly pH. If validated in independent populations and environments, this framework could guide processing-oriented breeding and industrial raw material selection by prioritizing stenospermocarpy and, secondarily, favorable pH profiles.

5. Conclusions

This study presents the largest systematic evaluation of lychee processing quality to date, phenotyping 301 genetically diverse accessions under uniform conditions and establishing a “structural constraint–physiological modulation” two-tier regulatory hierarchy. Kernel ratio is the dominant structural constraint on edible ratio (R2 = 0.6699) and the combined inedible fraction serves as the basal limiting factor for juice yield (R2 = 0.4262), with the high coefficient of variation in kernel ratio (CV = 40.4%) indicating substantial genetic potential for improving edible proportion through stenospermocarpy-targeted breeding. After controlling for structural variation, physiological traits contribute an independent 9.2% of explained variance to juice yield (ΔR2 = 0.092, p < 0.001), with pH emerging as the primary positive physiological predictor (β = 0.322, p < 0.001), potentially reflecting pH-dependent modulation of cell wall pectin solubility and extraction efficiency, whereas soluble solids content exhibits only a negligible negative effect (β = −0.064), indicating that high sugar content is not a priority target for processing-oriented breeding. The Integrated Ideotype Score (IIS) further provides an objective, regression-weighted framework for multi-trait germplasm ranking, with elite accessions including ‘10_269’, ‘Yujinqiu’ and ‘Nuomici’ combining edible ratio >75% with juice yield >40% and representing priority candidates for dual-purpose fresh and processing applications. Taken together, these findings suggest that, if validated in multi-site, multi-year trials, this framework prioritizes stenospermocarpy improvement and, secondarily, favorable pH profiles to guide processing-oriented breeding and industrial raw material selection in lychee and potentially other non-climacteric subtropical fruits (Figure S5).

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/horticulturae12091098/s1, Table S1. Details of the 301 lychee accessions evaluated in this study. Table S2. Number of accessions by origin and maturity stage. Table S3. ANOVA effect sizes of origin and maturity on edible ratio and juice yield. Table S4. Pairwise Pearson correlation coefficients (r) and corresponding p-values among eight fruit-quality traits across 301 lychee accessions. Table S5. Principal component analysis results. Table S6. VIF diagnostics for regression model. Table S7. Hierarchical regression summary for juice yield and PJE. Figure S1. Boxplots of edible ratio and juice yield across different origins. Figure S2. Correlation network analysis of fruit quality traits. Figure S3. Diagnostic plots for the full regression model. Figure S4. Distribution of IIS across 301 accessions and top 10 ranked varieties. Figure S5. Conceptual summary of the “structural constraint-physiological modulation” two-tier regulatory hierarchy for lychee processing quality.

Author Contributions

Methodology, H.L., Y.J., F.S., Y.W. and H.H.; investigation, H.L., Y.J., F.S., Y.W. and H.H.; writing—original draft, H.L.; writing—review and editing, H.L.; supervision, Z.H. and Q.Y.; project administration, Z.H. and Q.Y.; funding acquisition, Q.Y. All authors have read and agreed to the published version of the manuscript.

Funding

This work was funded by the Guangdong Provincial Financial Special Project for Seed Industry Revitalization Initiative (2025-NBH-00-001) and Guangdong Province Modern Agricultural Industry Technology System Innovation Team Construction Project (2026CXTD19).

Institutional Review Board Statement

Not applicable.

Informed Consent Statement

Not applicable.

Data Availability Statement

The original contributions presented in this study are included in the article/Supplementary Material. Further inquiries can be directed to the corresponding authors.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Liang, M.; He, Z.; Xiao, S.; Meng, X. Unraveling the mechanisms and technologies to combat postharvest deterioration in litchi. J. Agric. Food Res. 2026, 27, 102860. [Google Scholar] [CrossRef] [Scilit]
  2. De Oliveira, M.S.; Bordin, D.; de Souza, V.R.; de Oliveira, A.P.; de Oliveira, M.V.M.; dos Santos, G.R. Increasing the Brazilian Lychee Production: A Strategy Based on the Experience of the Largest Producer Countries. Horticulturae 2024, 10, 1301. [Google Scholar] [CrossRef] [Scilit]
  3. Cao, Y.; Jiang, Y.; Gao, H.; Chen, H.; Fang, X.; Mu, H.; Tao, F. Development of a model for quality evaluation of litchi fruit. Comput. Electron. Agric. 2014, 106, 49–55. [Google Scholar] [CrossRef] [Scilit]
  4. Yan, Q.; Feng, J.; Chen, J.; Wen, Y.; Jiang, Y.; Mai, Y.; Huang, K.; Liu, H.; Shi, F. Comprehensive genomic and phenotypic analyses reveal the genetic basis of fruit quality in litchi. Genome Biol. 2025, 26, 222. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Yao, P.; Gao, Y.; Simal-Gandara, J.; Farag, M.A.; Chen, W.; Yao, D.; Delmas, D.; Chen, Z.; Liu, K.; Hu, H. Litchi (Litchi chinensis Sonn.): A comprehensive review of phytochemistry, medicinal properties, and product development. Food Funct. 2021, 12, 9527–9548. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Zhao, L.; Hu, Z.Y.; Yu, X.L.; Wu, Z.X. Processed products from litchi and longan and their processing technology in China. Acta Hortic. 2014, 90, 379–384. [Google Scholar] [CrossRef] [Scilit]
  7. Lal, N.; Singh, A.; Kumar, A.; Pandey, S. Assessment of variability, correlation and path analysis for the selection of elite clones in Litchi based on certain traits. Erwerbs-Obstbau 2023, 65, 1747–1754. [Google Scholar] [CrossRef] [Scilit]
  8. Vallarino, J.G.; Hong, J.; Wang, S.; Wang, X.; Sade, N.; Orf, I.; Zhang, D.; Shi, J.; Shen, S.; Cuadros-Inostroza, Á. Limitations and advantages of using metabolite-based genome-wide association studies: Focus on fruit quality traits. Plant Sci. 2023, 333, 111748. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Bizeti, H.S.; Carvalho, C.G.P.; Souza, J.R.P.; Destro, D. Path analysis under multicollinearity in soybean. Braz. Arch. Biol. Technol. 2004, 47, 669–676. [Google Scholar] [CrossRef] [Scilit]
  10. Berardini, N.; Knödler, M.; Schieber, A.; Carle, R. Utilization of mango peels as a source of pectin and polyphenolics. Innov. Food Sci. Emerg. Technol. 2005, 6, 442–452. [Google Scholar] [CrossRef] [Scilit]
  11. Jiao, Y.; Liu, X.; Bi, J.; Wu, X.; Zhou, M.; Zeng, M. Suitability evaluation of flat peach cultivars for fresh juice processing. Food Sci. 2015, 36, 41–47. [Google Scholar]
  12. Sharma, H.P.; Patel, H.; Sugandha. Enzymatic Added Extraction and Clarification of Fruit Juices-A Review. J. Food Sci. Technol. 2017, 54, 1109–1121. [Google Scholar]
  13. Tian, W.; Li, Z.; Wang, L.; Sun, S.; Wang, D.; Wang, K.; Wang, G.; Liu, Z.; Lu, X.; Feng, J.; et al. Comprehensive evaluation of apple germplasm genetic diversity on the basis of 26 phenotypic traits. Agronomy 2024, 14, 1264. [Google Scholar] [CrossRef] [Scilit]
  14. Costa, C.D.S.R.; de Lima, M.A.C.; Neto, F.P.L.; Costa, A.E.D.S.; Vilvert, J.C.; Martins, L.S.S.; Musser, R.D.S. Genetic parameters and selection of mango genotypes using the FAI-BLUP multitrait index. Sci. Hortic. 2023, 317, 111003. [Google Scholar] [CrossRef] [Scilit]
  15. Cohen, J.; Cohen, P.; West, S.G.; Aiken, L.S. Applied Multiple Regression/Correlation Analysis for the Behavioral Sciences, 3rd ed.; Lawrence Erlbaum Associates: Mahwah, NJ, USA, 2003. [Google Scholar]
  16. Arlot, S.; Celisse, A. A survey of cross-validation procedures for model selection. Stat. Surv. 2010, 4, 40–79. [Google Scholar] [CrossRef] [Scilit]
  17. Mac Nally, R. Regression and model-building in conservation biology, biogeography and ecology: The distinction between—And reconciliation of—’predictive’ and ‘explanatory’ models. Biodivers. Conserv. 2000, 9, 655–671. [Google Scholar] [CrossRef] [Scilit]
  18. Hair, J.F.; Black, W.C.; Babin, B.J.; Anderson, R.E. Multivariate Data Analysis, 7th ed.; Pearson: Upper Saddle River, NJ, USA, 2010. [Google Scholar]
  19. Raj, D.; Sharma, P.; Vaidya, D. Effect of blending and storage on quality characteristics of blended sand pear-apple juice beverage. J. Food Sci. Technol. 2011, 48, 102–105. [Google Scholar] [CrossRef] [Scilit] [PubMed][Green Version]
  20. Miguel, G.; Fontes, C.; Martins, D.; Neves, A.; Antunes, D.; Gomes, S.; Cavaco, A.M.; Duarte, J.; Rodrigues, M.; Trindade, H. Fruit Quality Traits and Genotypic Characterization in a Pomegranate Ex Situ Collection. Agriculture 2021, 11, 482. [Google Scholar] [CrossRef] [Scilit]
  21. Hu, G.; Feng, J.; Xiang, X.; Wang, J.; Salojarvi, J.; Liu, C.; Wu, Z.; Zhang, J.; Liang, X.; Jiang, Z.; et al. Two divergent haplotypes from a highly heterozygous lychee genome suggest independent domestication events for early and late-maturing cultivars. Nat. Genet. 2022, 54, 73–83. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Xie, H.; Zheng, Y.; Xue, M.; Huang, Y.; Qian, D.; Zhao, M.; Li, J. DNA methylation-mediated ROS production contributes to seed abortion in litchi. Mol. Hortic. 2024, 4, 12. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Xie, D.R.; Ma, X.S.; Rahman, M.Z.; Yang, M.C.; Huang, X.; Li, J.; Wang, H. Thermo-sensitive sterility and self-sterility underlie the partial seed abortion phenotype of Litchi chinensis. Sci. Hortic. 2019, 247, 156–164. [Google Scholar] [CrossRef] [Scilit]
  24. Mafrica, R.; Gattuso, A.; Mafrica, D.; De Bruno, A.; Poiana, M. Influence of rootstock on growth, yield, and fruit quality of the ‘Femminello’ bergamot (Citrus bergamia Risso & Poit.). Agriculture 2026, 16, 405. [Google Scholar] [CrossRef] [Scilit]
  25. Brummell, D.A.; Harpster, M.H. Cell wall metabolism in fruit softening and quality and its manipulation in transgenic plants. Plant Mol. Biol. 2001, 47, 311–340. [Google Scholar] [CrossRef] [Scilit]
  26. Pattarapisitporn, A.; Noma, S. Alternative solvents for pectin extraction: Effects of extraction agents on pectin structural characteristics and functional properties. Foods 2025, 14, 2644. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  27. Krokida, M.K.; Maroulis, Z.B.; Saravacos, G.D. Rheological properties of fluid fruit and vegetable puree products: Compilation of literature data. Int. J. Food Prop. 2001, 4, 179–200. [Google Scholar] [CrossRef] [Scilit]
  28. Jiang, Y.; Yao, L.; Lichter, A.; Li, J. Postharvest biology and technology of litchi fruit. J. Food Agric. Environ. 2003, 1, 76–81. [Google Scholar]
  29. Wei, Y.Z.; Zhang, H.N.; Li, W.C.; Xie, J.H.; Wang, Y.C.; Liu, L.Q.; Shi, S.Y. Phenological growth stages of lychee (Litchi chinensis Sonn.) using the extended BBCH-scale. Sci. Hortic. 2013, 161, 273–277. [Google Scholar] [CrossRef] [Scilit]
  30. Xie, J.; Qin, Z.; Pan, J.; Li, J.; Li, X.; Khoo, H.E.; Dong, X. Melatonin treatment improves postharvest quality and regulates reactive oxygen species metabolism in “Feizixiao” litchi based on principal component analysis. Front. Plant Sci. 2022, 13, 965345. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Perotti, M.F.; Posé, D.; Martín-Pizarro, C. Non-climacteric fruit development and ripening regulation: ‘The phytohormones show’. J. Exp. Bot. 2023, 74, 6237–6253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Piepho, H.P.; Möhring, J.; Melchinger, A.E.; Büchse, A. BLUP for phenotypic selection in plant breeding and variety testing. Euphytica 2008, 161, 209–228. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Geographic distribution and maturity composition of the 301 lychee accessions. (A) Global distribution map of lychee accessions. Red gradient shading corresponds to the quantity of germplasm collected from each producing area, with representative varieties labeled. (B) Representative mature lychee fruits exhibiting natural variation in fruit size and pericarp color across tested materials. (C) Bar plot showing absolute counts of accessions divided into four maturity stages. (D) Stacked percentage bar chart displaying the proportional maturity composition of each geographical origin. Each bar is labeled with the total number of accessions (n) for each geographical origin. Note: the maturity composition shown reflects only the accessions included in this study and may not represent the full diversity of the respective regions, particularly for origins with small sample sizes (e.g., Laos, n = 1). Moreover, foreign accessions were cultivated in Guangzhou under local climatic conditions, which may alter their ripening phenology relative to their native environments.
Horticulturae 12 01098 g001
Figure 2. Phenotypic characterization of edible ratio and juice yield for 301 lychee accessions. (A,B) Frequency distribution histograms of edible ratio (A) and juice yield (B) based on biological replicate observations; the vertical axis indicates the number of individual observations per bin. (C,D) Box plots of edible ratio (C) and juice yield (D) across four maturity stages. (E) Scatter plot showing the correlation between edible ratio and juice yield. The red line represents the linear regression fit, and the gray shaded area indicates the 95% confidence interval. (F) Dashed lines represent the overall population means and serve solely as visual references; they are not classification cutoffs. The four clusters were designated according to their bivariate centroids.
Horticulturae 12 01098 g002
Figure 3. Population variation in eight morphological and fruit quality traits in 301 lychee accessions. (A) Frequency histograms for peel ratio, kernel ratio, SSC, pH, fruit weight, and inedible fraction. (B) Coefficients of variation for all eight evaluated traits. CV, coefficient of variation; SSC, soluble solids content.
Horticulturae 12 01098 g003
Figure 4. Correlation matrix and PCA of seven fruit quality and morphological traits in 301 lychee accessions. (A) Correlation heatmap for all evaluated traits, with color intensity and circle size proportional to correlation coefficients. Exact Pearson’s r-values and p-values are provided in Supplementary Table S4. (B) Scree plot showing the proportion of total variance explained by each principal component. (C) PCA loading biplot displaying trait contributions to PC1 (Dim1, 50.2%) and PC2 (Dim2, 15.7%). (D) PCA score plot colored by germplasm geographical origin, with 95% confidence ellipses for each origin group. SSC, soluble solids content; PC, principal component.
Horticulturae 12 01098 g004
Figure 5. Linear regression scatter plots revealing pairwise associations between key fruit processing traits of 301 lychee accessions. (A) Two panels of linear regression analysis for edible ratio against peel ratio and kernel ratio, respectively. (B) Four panels of linear regression analysis for juice yield versus inedible fraction, SSC (soluble solids content), pH, and fruit weight, respectively; fitted linear lines and corresponding statistical parameters are labeled in each subplot. The red line represents the linear regression fit, and the gray shaded area indicates the 95% confidence interval.
Horticulturae 12 01098 g005
Figure 6. Hierarchical regression dissecting structural and physiological drivers of juice yield and processing efficiency (PJE) in 301 lychee accessions. (A) Standardized regression coefficients (β) with 95% CI for juice yield (blue) and PJE (red), grouped into structural (inedible fraction) and physiological (SSC, pH, fruit weight) predictors. Significance levels: ** p < 0.01, *** p < 0.001. (B) R2 comparison among three models: M1 (structural), M2 (full), and PJE. ΔR2 (M1→M2) = 0.092, p < 0.001. PJE, pulp juice efficiency; SSC, soluble solids content; CI, confidence interval.
Horticulturae 12 01098 g006
Table 1. Descriptive statistics of quality traits.
TraitMeanSDCVMinMax
Edible ratio (%)67.397.2110.7%44.3484.41
Juice yield (%)30.3411.2036.9%8.2956.99
Inedible fraction (%)32.617.2122.1%15.5955.66
Peel ratio (%)20.534.1720.3%9.6832.86
Kernel ratio (%)12.084.8840.4%1.6628.60
SSC (°Brix)16.901.539.1%11.8721.77
pH2.940.5017.1%1.754.26
Fruit weight (g)21.557.5735.1%6.0465.06
Descriptive statistics of eight quality traits across 301 lychee accessions. CV, coefficient of variation; SD, standard deviation; SSC, soluble solids content.
Table 2. Top 5 accessions ranked by Integrated Ideotype Score (IIS).
VarietyEdible RatioJuice YieldInedibleSSCpHFruit WeightIIS
10_26982.6449.6417.3618.273.7138.001.67
Yujinqiu82.9450.8417.0616.803.9919.451.58
Dadingxiang74.0150.6325.9912.733.9241.481.57
Houxian76.1956.9923.8115.233.7645.151.56
Nuomici84.4156.0715.5916.773.5723.851.52
Higher IIS indicates better combined performance in structural and physiological traits. Accession labels with numerical prefixes (e.g., 10_269) represent hybrid progenies from controlled crosses; named accessions are traditional cultivars or landraces.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.