Article

Transcriptomic Analysis of Water Control Regulating Citrus Fruit Size and Citric Acid Accumulation


1
Institute of Citrus Research, Zhejiang Academy of Agricultural Sciences, Taizhou 318026, China
2
Taizhou Vocational College of Science & Technology, Taizhou 318020, China
*
Author to whom correspondence should be addressed.
Horticulturae 2026, 12(7), 818; https://doi.org/10.3390/horticulturae12070818
Submission received: 27 April 2026 / Revised: 25 June 2026 / Accepted: 2 July 2026 / Published: 3 July 2026
(This article belongs to the Special Issue Sustainable Approaches for Fruit Quality of Horticultural Crops)

Abstract

Soil moisture plays a crucial regulatory role in determining the size and quality of citrus fruits. This study analyzed the fruit size and quality of citrus under different soil moisture conditions, including severe drought (SD), moderate drought (MD), and control (CK). Under drought stress, the fruit weight, longitudinal diameter, and transverse diameter of citrus fruits were significantly lower than those of the control. The content of soluble solids and titratable acid in fruits under drought stress was significantly higher than that of the control. Transcriptome sequencing revealed that compared with CK, there were 1186 differentially expressed genes in MD, including 414 up-regulated genes and 772 down-regulated genes; and 2315 differentially expressed genes in SD, including 1143 up-regulated genes and 1172 down-regulated genes. The differentially expressed genes were significantly enriched in cellular processes, metabolic processes, and plant hormone signal transduction. The down-regulated expression of auxin and gibberellin biosynthesis genes (YUC10, GA20OX1, GA2OX1, and GA20OX2) and signal transduction-related genes (AUX/IAA13, SAUR32, GH3.1, and ARRs), and the up-regulated expression of cytokinin decomposition gene (CKX5) may be associated with reduced fruit size under drought conditions. The up-regulated expression of citric acid synthesis genes (PEPC2 and PEPCK1) and vacuolar transporters (PH1, PH4, PH8, and VHA-c3) may be associated with pronounced accumulation of citric acid in citrus under drought stress. In conclusion, water control regulated fruit size and acidity by modulating phytohormone metabolism and signaling, along with the synthesis and transport of citric acid.

1. Introduction

Citrus is among the world’s most economically and nutritionally advantageous fruit crops, cultivated extensively across 169 countries and regions. Citrus fruits and peels are abundant in soluble sugars, organic acids, flavonoids, vitamins, mineral nutrients (including potassium, calcium, magnesium, phosphorus), and dietary fiber, which confer significant health benefits to humans [1]. Soil moisture serves as a key environmental factor that significantly influences both the yield and quality of citrus fruits. The issue of water shortage exists in most citrus-producing regions [2]. In southern China, the distribution of precipitation in terms of both time and space is extremely uneven, and seasonal droughts occur frequently, especially from July to September [3], a period that coincides with the critical stage of citrus fruit expansion, during which soil drought exerts significant adverse effects on both fruit yield and quality. In the mature stage, moderate drought stress inhibits the vegetative growth of fruit trees while promoting sugar accumulation in the fruits, thereby enhancing fruit quality [4,5]. While severe drought impaired water metabolism and photosynthetic activity in fruit trees, thereby limiting the accumulation of assimilates and ultimately reducing both fruit yield and quality [6]. Controlling environmental factors through the utilization of greenhouses is a crucial approach to cultivating high-quality citrus fruits [7,8]. Facility greenhouses with integrated water and fertilizer equipment prevent flowering frost damage, regulate diurnal temperature variation, and control soil moisture, thus improving citrus yield and quality by creating favorable growth conditions [8].
Fruit size is a complex agronomic and commercial trait influenced by a multitude of factors, including genetics, endogenous hormones, the environment, and cultivation measures [9,10,11,12]. Multiple pivotal quantitative trait loci, including fw2.2, fw3.2, FAS, LC, YABBY, and WOX transcription factor family, regulated cell proliferation and fruit size [13]. Phytohormones, including auxin, gibberellin (GA), cytokinin (CTK), and brassinosteroid (BR), regulate cell division and expansion. The elevated expression of auxin synthesis genes (MdTAR1 and MdYUCCA6), which increased endogenous auxin accumulation, constitutes the primary molecular determinant underlying the large-fruit mutant phenotype in apple [12]. Over-expression of CsMYB77 in citrus activates the expression of PIN5, thereby promoting the reduction in free indole-3-acetic acid content and leading to a significant decrease in fruit size [9]. Genes involved in cell division and the cell cycle, such as CYCD3, HISTONE H4, and WEE1, regulate fruit size in tomatoes (Solanum lycopersicum) [14] and cucumber (Cucumis sativus) [15] by controlling cell numbers. Precise water and fertilizer management significantly increases fruit size and soluble solid content in pear [16] and citrus [17]. Manual fruit thinning significantly increases Ponkan (Citrus reticulata) fruit size by up-regulating the transcript levels of various auxin and gibberellin biosynthesis and signaling genes [10].
The content of soluble sugar and organic acid in citrus fruits is an important indicator of their intrinsic quality. Citric acid is the main organic acid in citrus fruits, accounting for 66–99% of the total acid [18]. The accumulation of citric acid in citrus fruits follows a pattern of first increasing during the fruit expansion stage and then decreasing during the ripening stage [19]. During the fruit expansion stage, the content of citric acid in citrus fruits rises rapidly, and it is degraded through the catalysis of ACO, IDH, GAD, and ACL as the fruits mature [20,21,22]. The accumulation of citric acid in citrus fruits is regulated by environmental factors such as temperature and moisture [3]. The content of citric acid in Ponkan fruits significantly increases by 40% to 90% under low-temperature conditions [7]. Under drought stress, the citric acid content in citrus fruits significantly increases, causing the fruits to become more acidic and their intrinsic quality to decline.
Soil moisture is closely related to the size of citrus fruits and the accumulation of sugar and acid. Preliminary findings show that improper irrigation reduces citrus fruit size and increases acidity. We hypothesize that soil moisture may regulate citrus fruit development and citric acid accumulation. To clarify the optimal soil moisture level for high-quality citrus fruits in facility greenhouses, an integrated fruit quality assessment and transcriptome sequencing of citrus across irrigation treatments was conducted in this study.

2. Materials and Methods

2.1. Plant Material

This experiment was conducted in the facility greenhouse of Zhejiang Citrus Research Institute (121°9′30″E, 28°38′36″N) from 2023 to 2024. The experimental material was a 5-year-old root-restricted ‘Himekoharu’ (Citrus reticulata) grafted on ‘Trifoliate Orange’ (Poncirus trifoliata) rootstock. The diameter of the root container was 80 cm, and the height was 60 cm. The cultivation substrate consisted of yellow soil, river sand, and mushroom residue in a volume ratio of 1:1:1, with the following physicochemical properties: pH 5.7; organic matter content 3.1% (w/w), available nitrogen, 107 mg/kg; available phosphorus, 81 mg/kg; and available potassium, 148 mg/kg.

2.2. Sample Processing and Collection

‘Himekoharu’ mandarin trees with a similar size and uniform growth vigor were selected. Three water control treatments were set up during the fruit expansion stage (July to August), including severe drought treatment SD (soil relative water content 45% ≤ T1 < 55%), moderate drought treatment MD (soil relative water content 55% ≤ T2 < 65%), and control (soil relative water content 75% ≤ control < 85%). The soil relative water content was measured by a soil moisture tester (ZD-1608, ZD instrument, Co., Ltd., Taizhou, China) at 9:00 am every day. Citrus trees were irrigated via drip irrigation systems, with irrigation frequency and volume dynamically adjusted based on real-time measurements of soil relative water content. Each treatment contained three replicates, with three trees in each replicate. In March 2024, fruit samples from each treatment were collected to measure fruit quality parameters. A total of eight fruits were randomly sampled from the outer canopy of each tree across four directions. Meanwhile, a subsample of citrus fruits was immediately sliced into small pieces, rapidly frozen in liquid nitrogen, and stored at −80 °C for subsequent RNA extraction.

2.3. Fruit Quality Determination

Fruit weight was measured using an electronic balance. Transverse diameter, longitudinal diameter, and peel thickness were measured with an electronic vernier caliper. Fruit color was assessed using a CR-400 colorimeter (Konica Minolta, Tokyo, Japan); total soluble solid (TSS) content was quantified with a PAL-1 refractometer (ATAGO, Tokyo, Japan), and titratable acidity (TA) was measured with a PLA–Easy ACID1 pH meter (ATAGO, Tokyo, Japan). Citric acid content was quantified by high-performance liquid chromatography (HPLC) on an LC-10A system (Shimadzu, Kyoto, Japan), and the vitamin C content was determined by 2,6-dichlorophenolindophenol titration.

2.4. RNA Extraction and Transcriptome Analysis

The total RNA of SD, MD, and CK citrus fruits was extracted using a plant total RNA extraction kit (Takara, Dalian, China). Each treatment contained three biological replicates with a mixture of pulp from three fruits. The integrity and concentration of RNA were determined by 1% agarose gel electrophoresis and NanoPhotometer® spectrophotometer (IMPLEN, Westlake Village, CA, USA), respectively. Sequencing was performed by Gene Denovo Biotechnology Company (Guangzhou, China). After removing adapters and low-quality reads, the clean reads were mapped to the citrus genome (http://citrus.hzau.edu.cn/download.php, accessed on 28 December 2024). Gene expression levels were calculated using fragment per kilobase of transcript per million mapped reads (FPKM) values. Differentially expressed genes (DEGs) were analyzed using DESeq (v1.20.0) software and screened based on a |log2fold change (FC)| ≥ 1 and a false discovery rate (FDR) value ≤ 0.05. DEGs were subsequently subjected to Gene Ontology (GO) functional enrichment and Kyoto Encyclopedia of Genes and Genomes (KEGG) pathway enrichment analyses. All DEGs were mapped to GO terms, and significantly enriched terms were identified using a hypergeometric test (Qvalue ≥ 0.05) against the genomic background. KEGG enrichment analysis identified significantly enriched metabolic and signaling pathways among DEGs relative to the genomic background. RNA-Seq data analysis followed our previous study [23]. Nine differentially expressed genes related to phytohormone signal transduction and citric acid accumulation were selected to verify the transcriptome data by fluorescent quantitative PCR (qRT-PCR). β-actin was used as the internal reference gene. qRT-PCR primers were designed with Primer 5.0 and are listed in Supplementary Table S1. qRT-PCR was performed as described previously [24].

2.5. Statistical Analysis

Data are presented as mean ± standard error (SE). Graphs were generated using GraphPad Prism 8. Treatment differences were analyzed by one-way ANOVA in SAS 8.1, followed by Duncan’s multiple range test (p < 0.05).

3. Results

3.1. The Effects of Water Control Treatments on the Size and Quality of Citrus Fruits

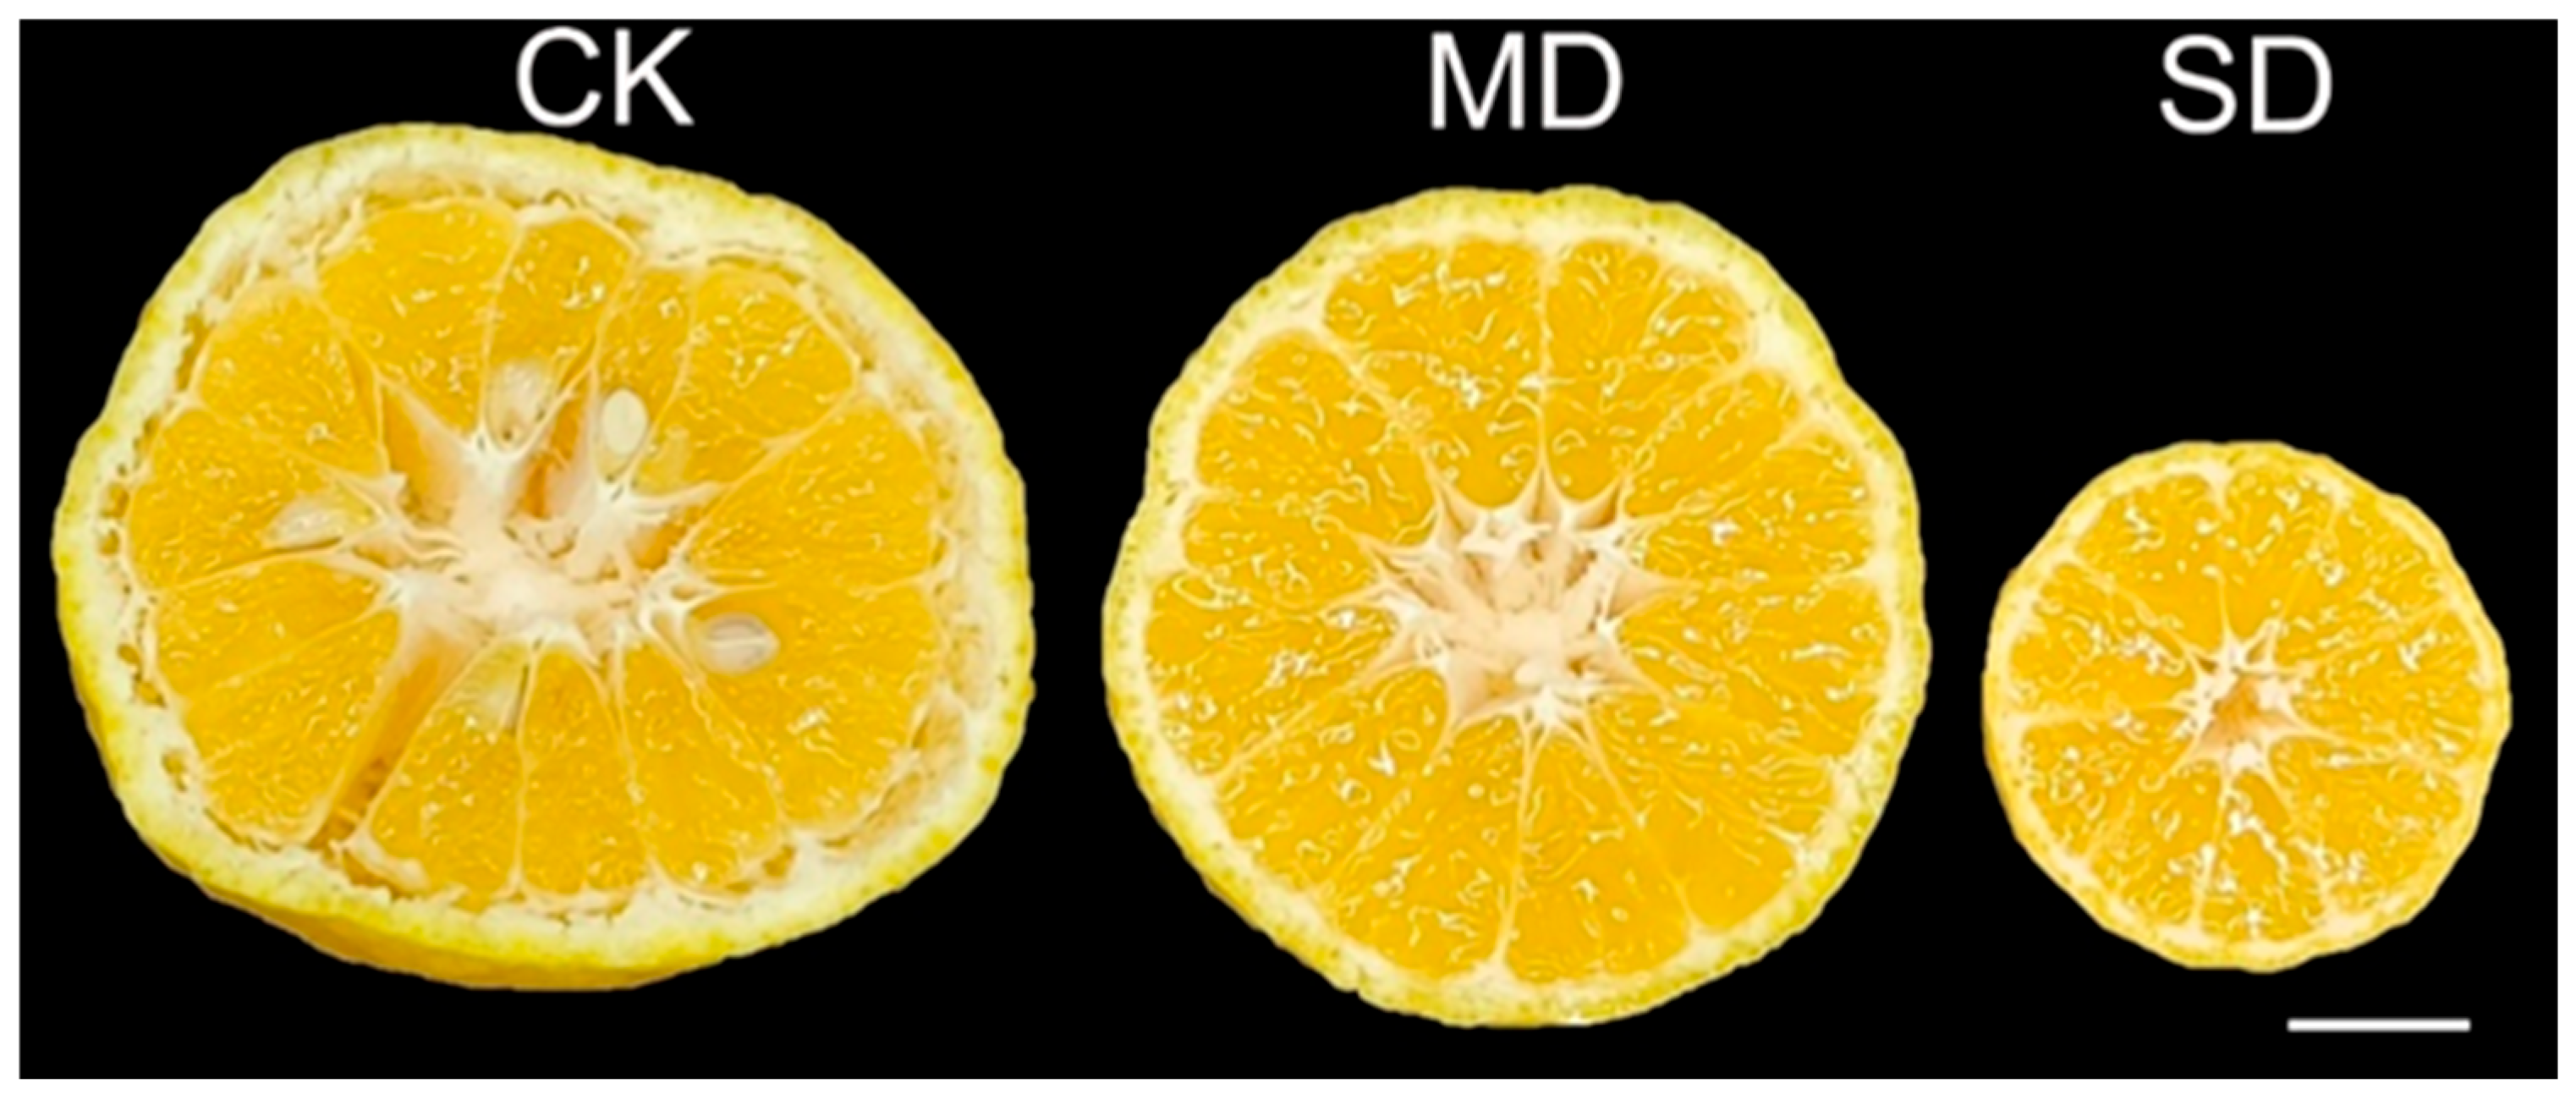
Water control treatment significantly altered the size and quality of citrus fruits. The L value of MD and SD was significantly higher than that of CK, and the b value of SD was significantly lower than that of CK (Figure 1 and Table 1). The single fruit weight of SD was 60.1 g, significantly lower than that of MD and CK. The longitudinal diameter of SD was 51.1 mm, significantly lower than that of MD and CK. The transverse diameters of MD and SD were 82.1 mm and 74.5 mm, respectively, both significantly lower than that of CK. The total soluble solid (TSS) content of MD and SD was 16.6% and 20.4%, respectively, significantly higher than that of CK. The total acid (TA) of MD and SD was 2.8 mg/100 mL and 5.3 mg/100 mL, respectively, significantly higher than that of CK. The solid-to-acid ratios (TAR) of MD and SD were 5.9 and 5.3, respectively, which were significantly lower than that of CK. The vitamin C (Vc) content of SD was 39.8 mg/100 mL, which was significantly higher than that of MD and CK (Table 1).

3.2. Screening of Differentially Expressed Genes

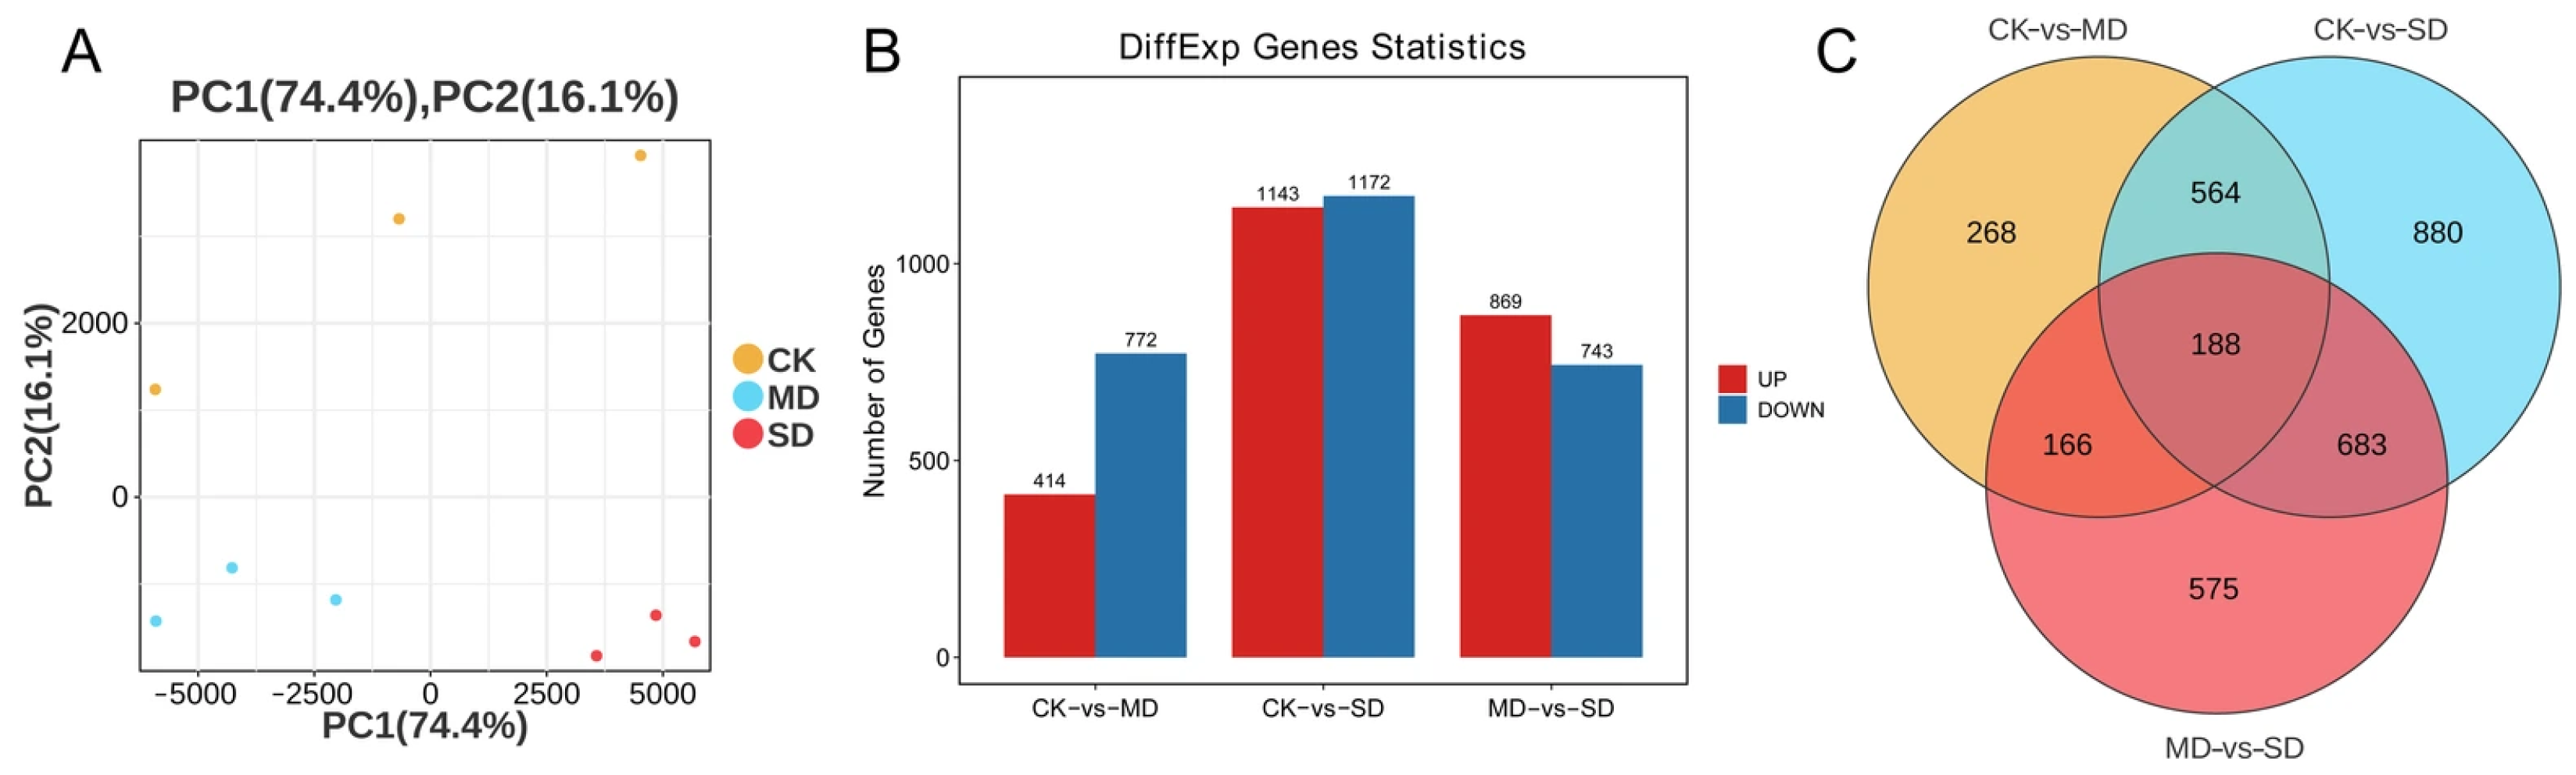
A total of 9 cDNA libraries were constructed for the citrus fruits of CK, MD, and SD, respectively. The sequencing obtained 42.1 GB, 39.6 GB, and 41.6 GB of clean reads, respectively. After removing ribosomal RNA, the data were compared with the reference genome, and the overall alignment rate exceeded 92%. 53% to 64% of the genes were aligned to the reference genome, and 766 new genes were discovered during the assembly (Supplementary Table S2). Principal component analysis (PCA) revealed that the first two principal components (PC1 and PC2) collectively account for 90.5% of the total variance (Figure 2A and Supplementary Table S3). Along PC1, samples from the severe drought stress (SD) group are distinctly separated from those of the moderate drought (MD) and control (CK) groups. DEGs were identified across all three treatment groups. Relative to the control (CK), the MD treatment exhibited 1186 DEGs, including 414 upregulated and 772 downregulated genes; whereas the SD treatment exhibited 2315 DEGs, including 1143 upregulated and 1172 downregulated genes. Furthermore, comparison between SD and MD revealed 1612 DEGs, including 869 upregulated and 743 downregulated genes. (Figure 2B and Supplementary Table S4). The Venn diagram analysis of DEGs identified 268 DEGs between the MD and CK treatments, 880 DEGs between the SD and CK treatments, 575 DEGs between the SD and MD treatments, and 188 DEGs commonly differentially expressed across all three treatment groups (Figure 3 and Supplementary Table S5).

3.3. Enrichment Analysis of Differentially Expressed Genes

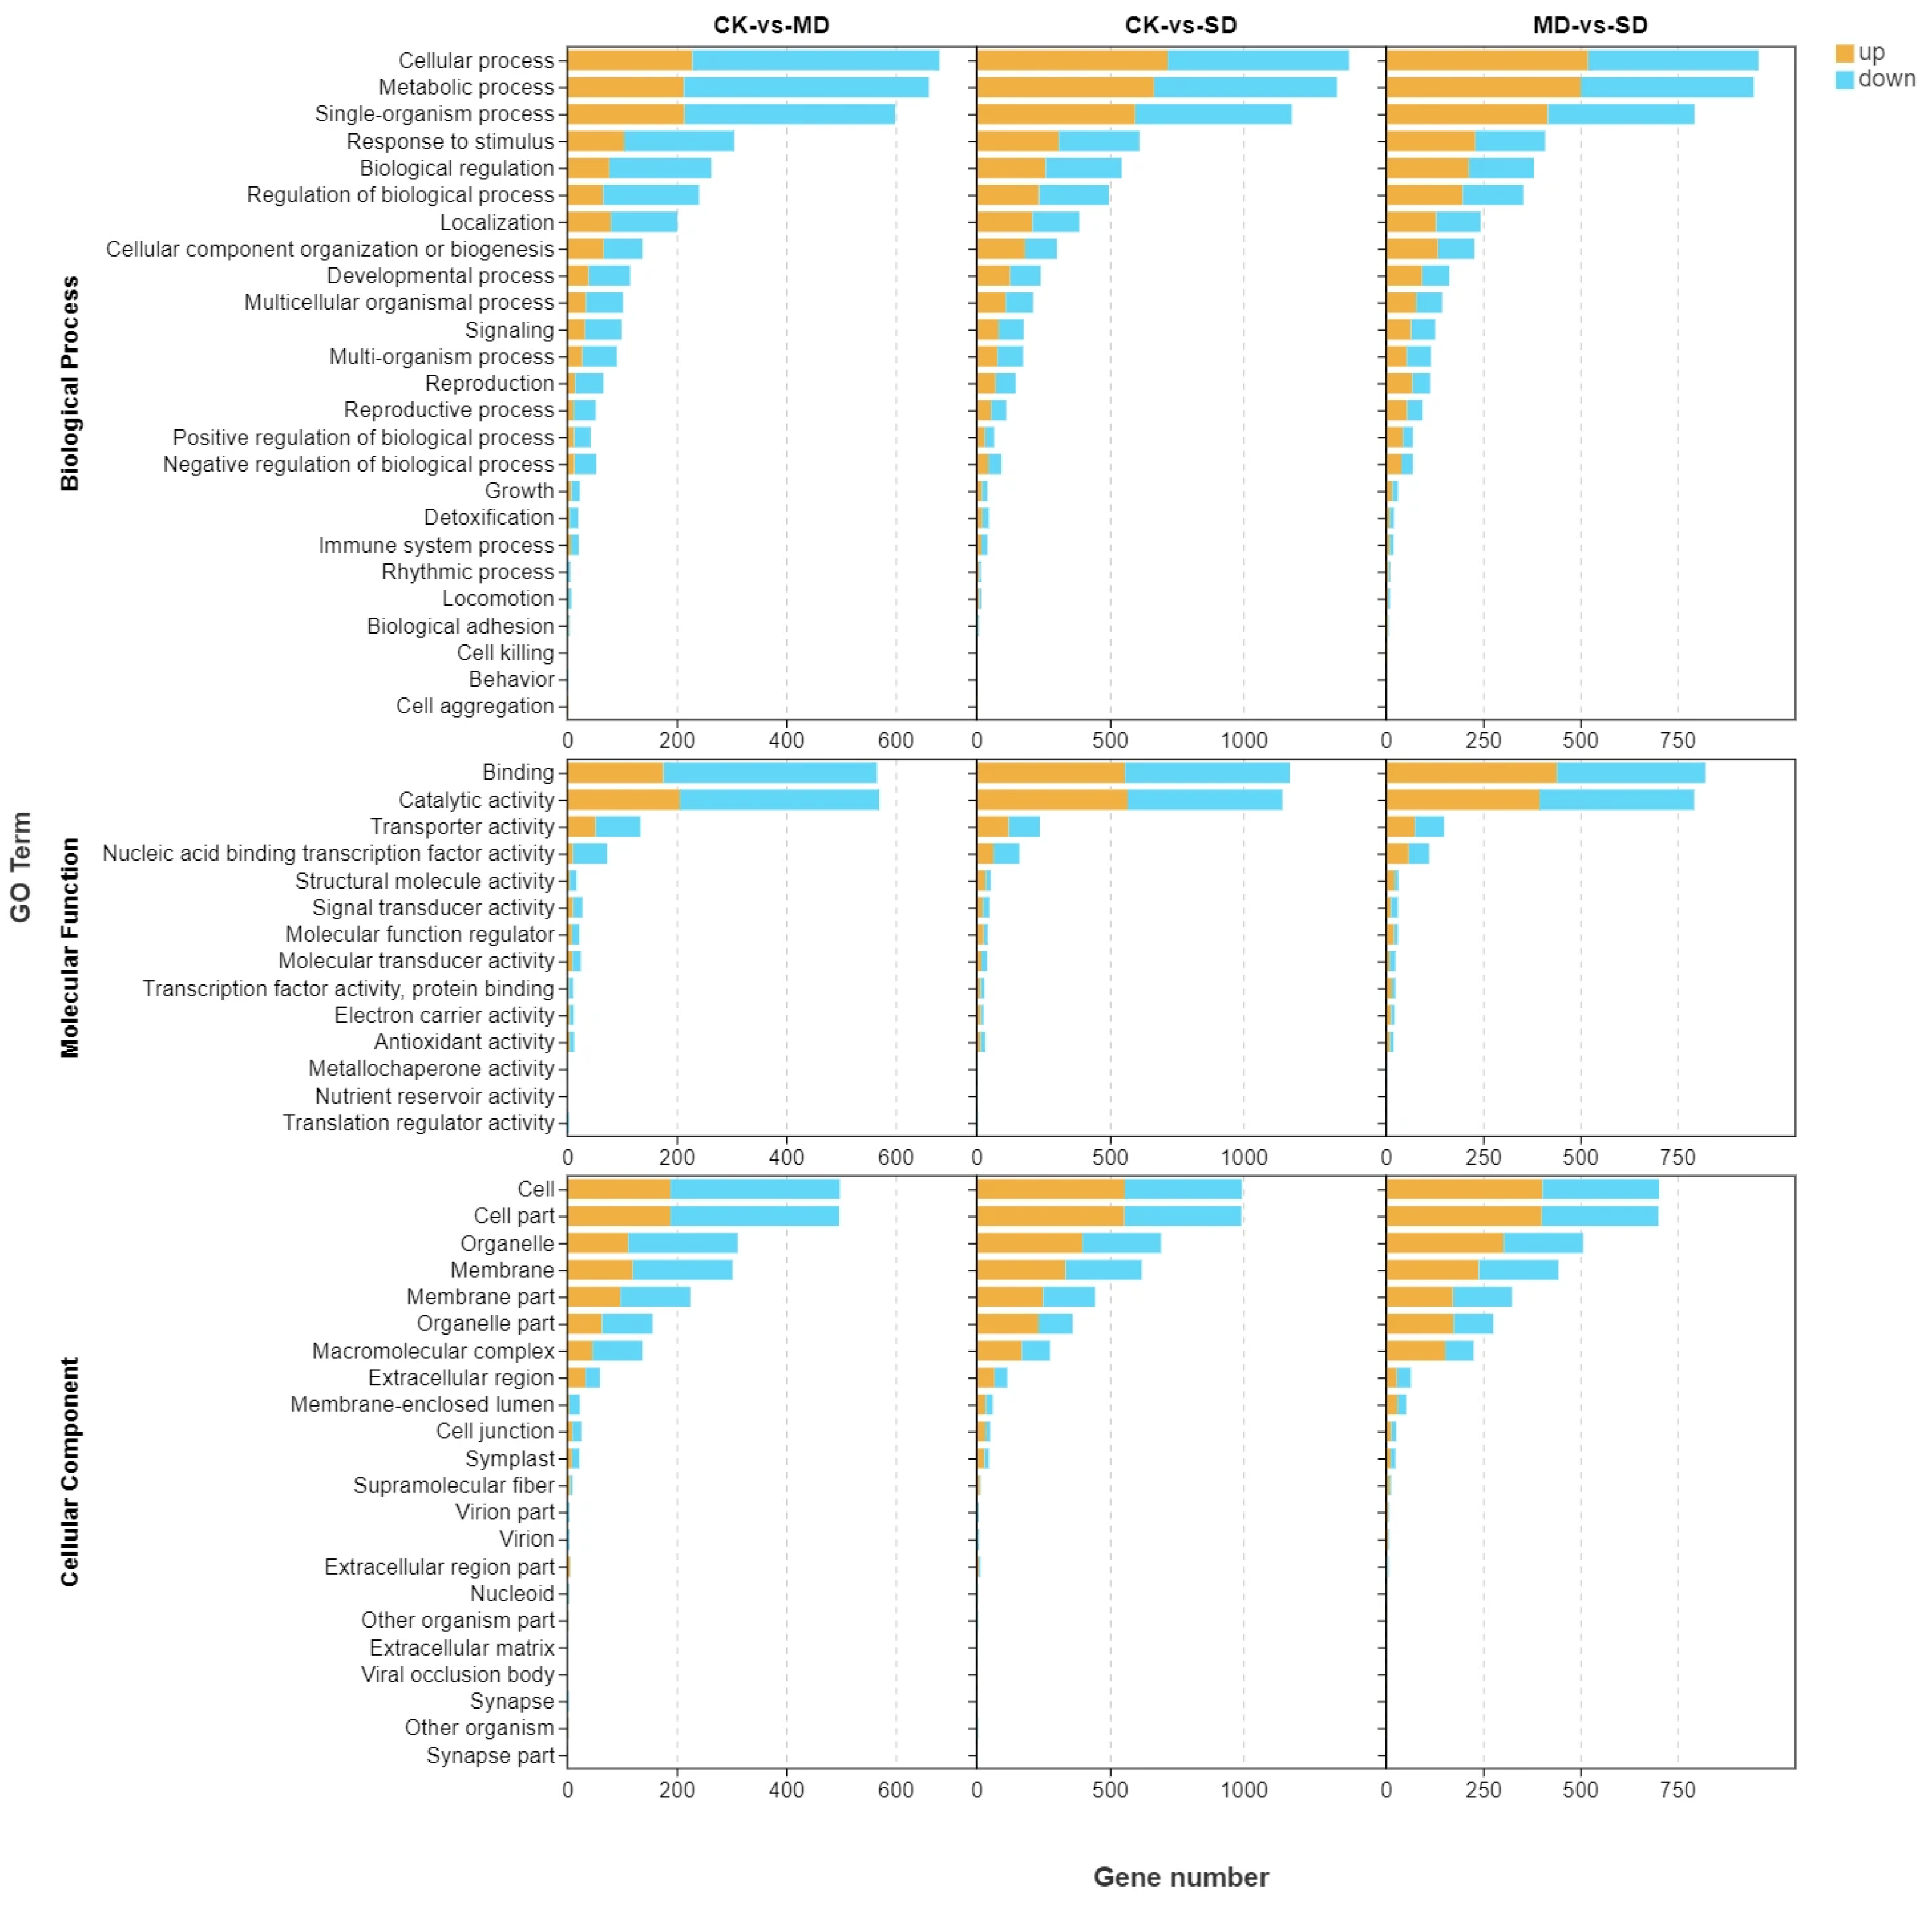
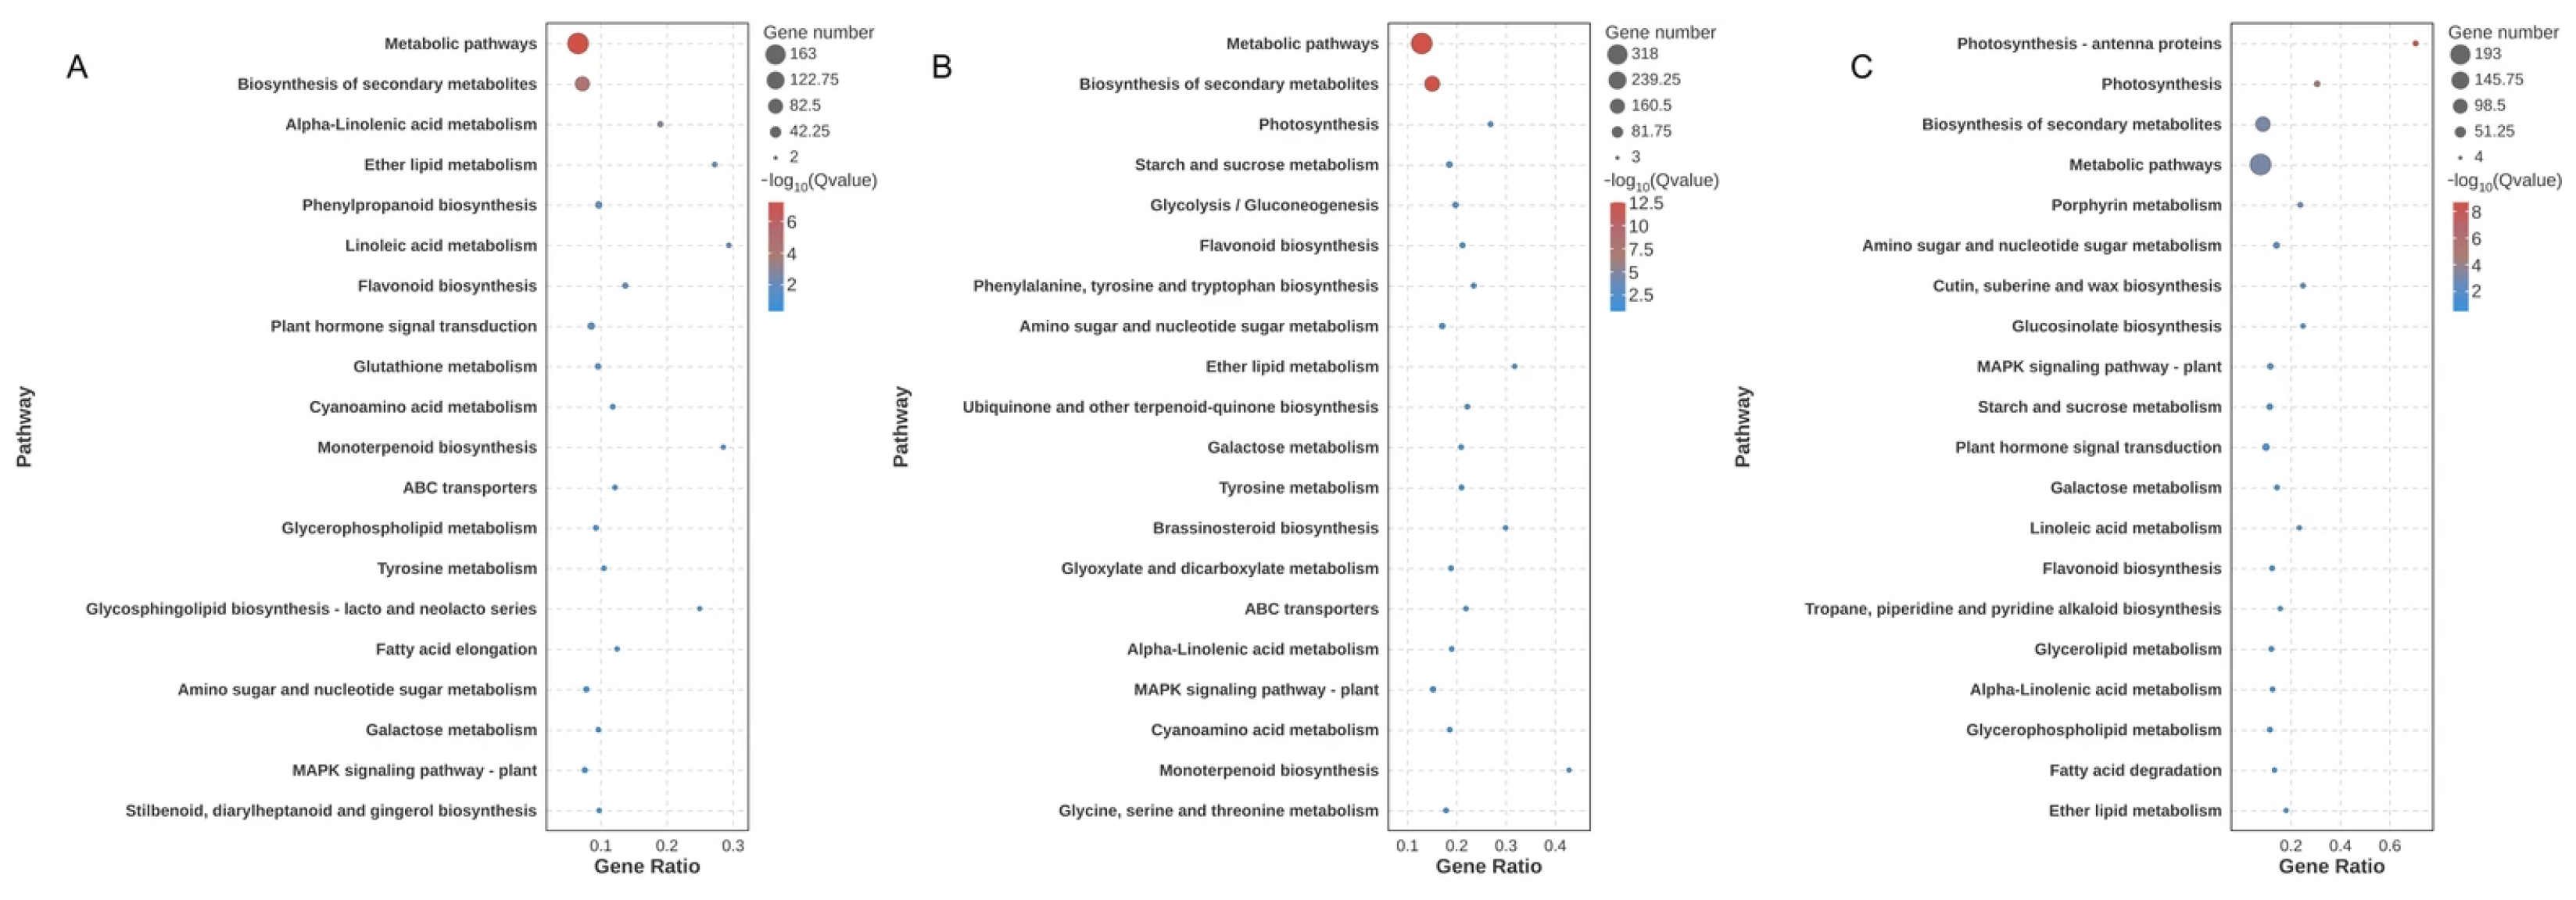
GO enrichment analysis was conducted on the differentially expressed genes among three pairwise comparisons (CK-vs-MD, CK-vs-SD, MD-vs-SD). The results revealed that DEGs were mainly enriched in biological processes such as cellular process, metabolic process, single-organism process, response to stimulus, and biological regulation; molecular functions such as binding, catalytic activity, transporter activity, and nucleic acid binding transcription factor activity; and cellular components such as cell, organelle, membrane, and macromolecular complex. Under severe drought (SD), the upregulation of stress-responsive pathways and downregulation of growth/developmental processes become more pronounced, while moderate drought (MD) elicits a more balanced response (Figure 3 and Supplementary Table S6). The KEGG enrichment analysis across three pairwise comparisons revealed distinct metabolic reprogramming under different drought intensities. Under moderate drought (CK-vs-MD), the most enriched pathways include “Metabolic pathways”, “Biosynthesis of secondary metabolites”, “Alpha-Linolenic acid metabolism”, “Ether lipid metabolism” and “Phenylpropanoid biosynthesis”. Under severe drought (CK-vs-SD), a broader and stronger activation is observed, with “Photosynthesis” and “Starch and sucrose metabolism” showing high gene ratios and significance, alongside “Flavonoid biosynthesis,” “Glycolysis/Gluconeogenesis”, and “Brassinosteroid biosynthesis”, reflecting a systemic shift toward energy conservation, osmotic adjustment, and hormone-mediated stress tolerance. In the MD-vs-SD comparison, the most dramatic changes occur in “Photosynthesis—antenna proteins” and “Photosynthesis”, along with enrichment of “Biosynthesis of secondary metabolites”, “MAPK signaling pathway—plant”, and “Plant hormone signal transduction”, suggesting that the transition from moderate to severe drought sharply suppresses photosynthetic light-harvesting and triggers massive secondary metabolism and stress signaling cascades (Figure 4 and Supplementary Table S7).
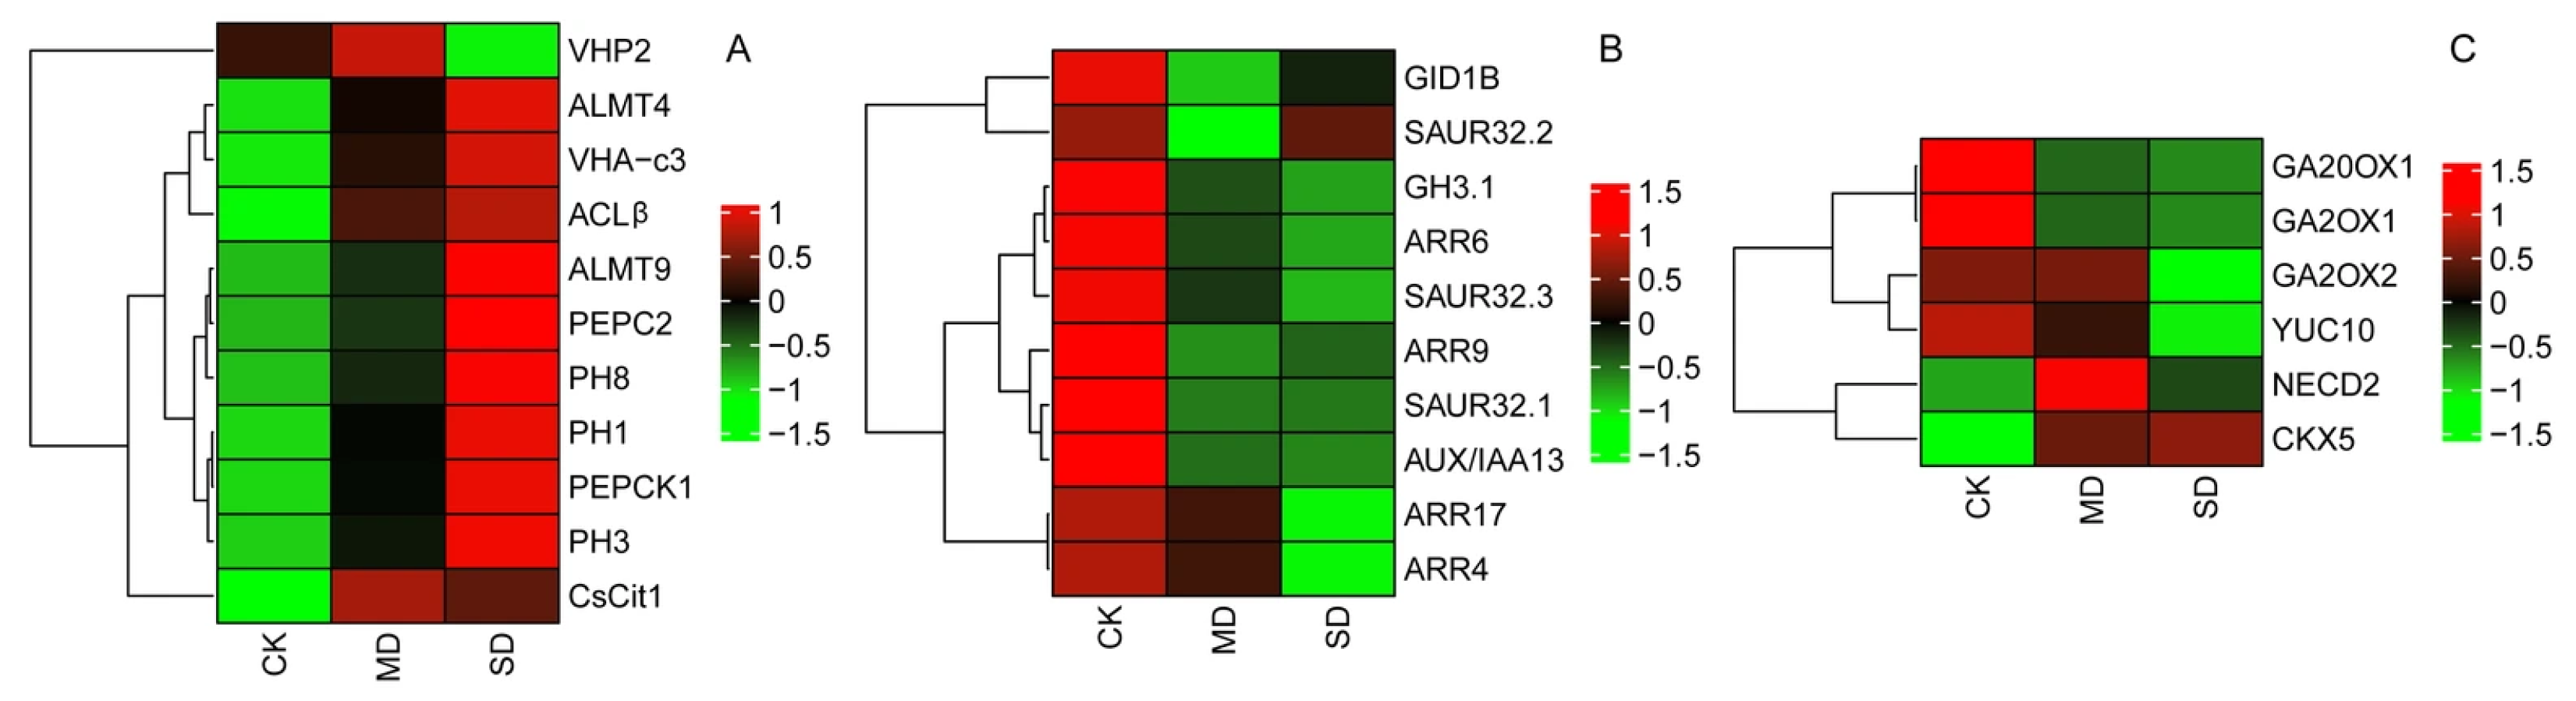
The analysis of genes related to citric acid metabolism and transport in citrus revealed that the expression levels of the genes encoding the citric acid synthesis-related enzymes, phosphoenolpyruvate carboxylase 2 (Cs_ont_2g026550) and phosphoenolpyruvate carboxykinase 1 (Cs_ont_3g012580.1), gradually increased with the severity of drought stress. The expression levels of three genes encoding P-type proton pumps (Cs_ont_1g017980, Cs_ont_6g024530, and Cs_ont_6g024620) also gradually increased with the severity of drought stress Figure 5A. KEGG enrichment analysis showed that 24 and 34 genes were enriched in the plant signal transduction pathway under moderate drought and severe drought stress, respectively. Among them, a gene encoding AUX/IAA13 in the auxin signaling pathway, three genes encoding SAUR (Cs_ont_7g012810, Cs_ont_5g005060, and Cs_ont_5g030560), and one gene encoding GH3.1 (Cs_ont_8g025760) were downregulated in the citrus fruits under drought treatment. Four genes encoding ARR (Cs_ont_5g046500, Cs_ont_3g009170, Cs_ont_7g003190, Cs_ont_7g025310) in the cytokinin signaling pathway were downregulated in the citrus fruits under drought treatment Figure 5B. Meanwhile, the expression of three gibberellin synthesis genes, including GA20OX1, GA2OX1, and GA2OX2 (Cs_ont_9g024810, Cs_ont_2g002160, Cs_ont_9g000810), and the auxin synthesis gene YUC10 (Cs_ont_5g009040) was down-regulated under drought treatment, while the expression of the abscisic acid synthesis gene NCED2 (Cs_ont_2g002030) and the cytokinin degradation gene CKX5 (Cs_ont_3g003070) was up-regulated under drought treatment Figure 5C.
Figure 5. The heatmap of genes in the key pathway among normal (CK), moderate drought (MD), and severe drought (SD) fruits. (A) Citric acid metabolism and transport, (B) Phytohormone signal transduction, (C) Phytohormone metabolism.
Horticulturae 12 00818 g005

3.4. qRT-PCR Analysis of Different Expressed Genes

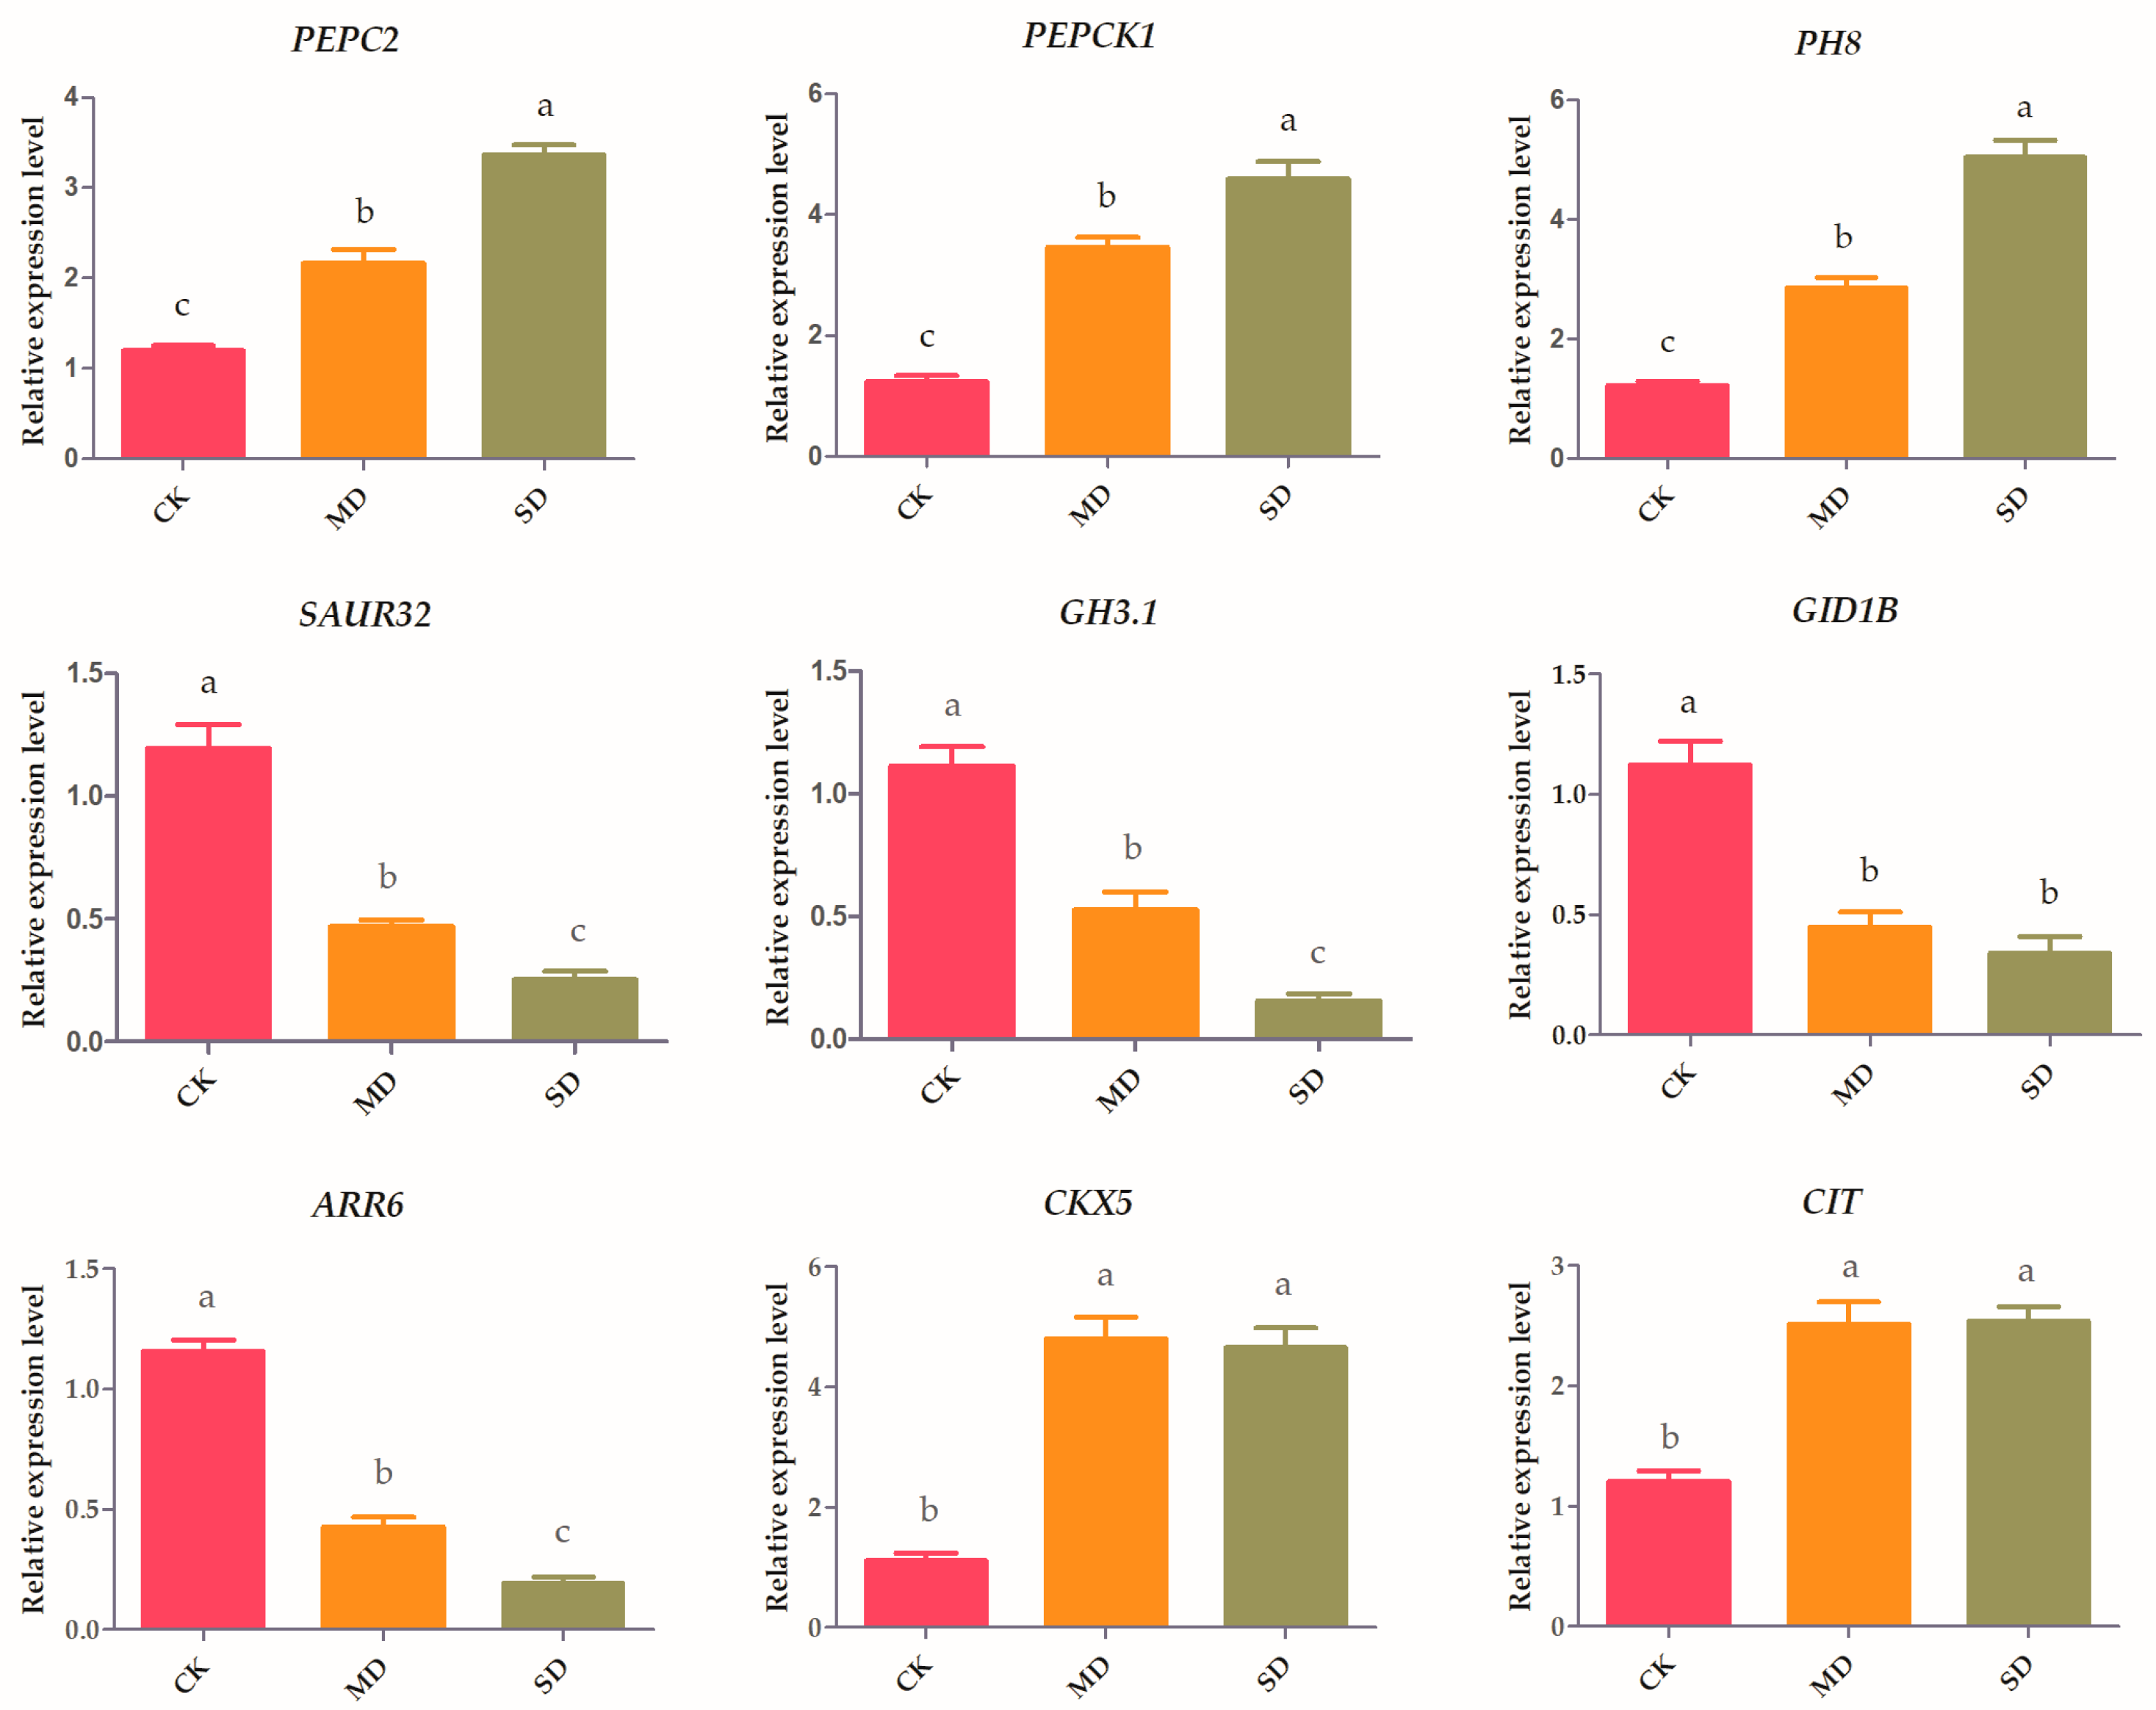
To verify the reliability of transcriptome data, nine differently expressed genes related to citric acid accumulation, phytohormone metabolism, and signaling (including PEPC2, PEPCK1, PH8, SURA32, GH3.1, GID1B, ARR6, CKX5, and CIT) were selected for expression analysis by qRT-PCR (Figure 6). The correlation coefficient between the transcriptome FPKM values of 9 differentially expressed genes and the qRT-PCR results was 0.85 (Supplementary Figure S1). Transcriptome data aligned with qRT-PCR results, confirming their reliability.

4. Discussion

Environmental factors, including light, temperature, and water, play a significant regulatory role in the fruit yield and quality. Fruits exhibit considerable differences in sensitivity to water stress across different fruit developmental stages. Drought stress at the fruit expansion stage markedly inhibited both fruit growth and final fruit size [25]. Water deficit during the citrus fruit expansion stage exerted significant impacts on fruit quality compared to other developmental stages. For instance, drought stress occurring in C. clementina during the fruit swelling stage (June to October) increases glucose and fructose accumulation while significantly decreasing sucrose concentration. [26]. Controlled irrigation applied during the citrus ripening stage significantly enhances the fruit soluble sugar content [27]. In this study, citrus fruits subjected to drought treatment during the fruit expansion stage exhibited significantly reduced fruit size compared to the control, while displaying markedly higher levels of total soluble solids and titratable acids. The SWEET gene family is an important sugar transporter involved in sugar accumulation in fruits [28,29]. The expression level of Sweet17 (Cs_ont_3g015160) in MD fruits was significantly higher than that in the control. GO and KEGG enrichment analysis revealed that DEGs were significantly enriched in plant hormone synthesis and signal transduction, cell division and cycle, citric acid metabolism, and storage. These results indicated that metabolic response alterations may play a critical regulatory role in mediating the effects of drought on fruit size and acidity.
The enlargement of fruits is the result of the coordinated regulation of cell division and cell expansion by auxin (IAA), cytokinin (CTK), and gibberellin (GA) [30]. After pollination, endogenous auxin concentration in fruit increased significantly, accompanied by the expression of auxin signal transduction-related transcription factors such as ARF and SAUR, which initiated cell division and differentiation and promoted fruit expansion [15,31]. In this study, Drought treatment significantly downregulated AUX/IAA, SAUR32, and GH3.1 expression in citrus fruit, which suggests that auxin signaling may be involved in soil moisture regulation of citrus fruit size. Cytokinin regulates fruit size primarily by increasing the total cell number during early developmental stages, facilitating cell division in the pulp, and ultimately influencing fruit size [32]. External application of substances exhibiting cytokinin activity, such as benzyladenine (BA) or forchlorfenuron (CPPU), directly stimulated cell division in young fruits, enhanced cell proliferation, and promoted fruit expansion [33]. Cytokinin dehydrogenase (CKX) catalyzed the oxidation of cytokinin and regulated the accumulation of cytokinin in plant cells. The expression level of CjCKX5 in the large-fruit mutant of jujube is significantly lower than that in the wild type. Heterologous overexpression of ZjCKX5 in tomato led to smaller fruits in transgenic plants [34]. Additionally, the expression of GmCKX13 was induced by drought stress [35]. In this study, the expression of the CKX5 gene in citrus fruit was up-regulated by factors of 2.8 and 3.0 under MD and SD treatments, respectively. Meanwhile, the expression levels of cytokinin regulators (ARR4, ARR6, ARR9, and ARR17) in drought-stressed citrus plants were significantly lower than those in the control. These results suggested that drought stress may induce the expression of CKX5, reduce the content of cytokinin in citrus fruits, and thereby inhibit the division of pulp cells, leading to a decrease in fruit size.
Citric acid is the predominant organic acid in citrus fruits, with its concentration serving as a critical indicator of fruit flavor. It is synthesized under the catalysis of phosphoenolpyruvate carboxylase (PEPC) and citrate synthase (CS) [36], and subsequently stored in vacuoles through the transport activity of vacuolar proton pumps [37,38,39]. Appropriate application of potassium significantly enhanced the activity and expression of CS and PEPC, and promoted the accumulation of citric acid [40]. In this study, the expression levels of PEPC2 and PEPCK1 in drought-treated citrus fruits were significantly higher than those in the control. Although this study did not measure PEPC activity, Jiang et al. reported a significant increase under 40-day mulch-based water control [27]. Overexpression of the GsPEPC4 gene from Gleditsia sinensis promoted organic acid accumulation and secretion [41]. Proton pumps play a crucial regulatory role in the transport and accumulation of citrate in citrus fruits. In citrus, PH8 is highly expressed in the juice sacs of fruits, and its expression level is significantly higher in high-acid varieties than in low-acid varieties [37]. Meanwhile, reducing the expression of PH8 can significantly decrease the accumulation of citric acid in citrus [39]. In navel oranges (C. sinensis), seasonal drought during fruit expansion promotes abscisic acid accumulation. The ABA-responsive factor AFB3 directly activates PH8 expression, increasing citric acid accumulation in vacuoles [3]. In this research, drought stress significantly induced the expression of genes encoding proton pumps (PH1, PH4, PH8, and VHA-c3). These results indicated that drought stress may promote both the synthesis and translocation of citric acid in citrus fruits, consequently leading to a marked increase in organic acid content.

5. Conclusions

Soil moisture content plays a crucial role in the formation of yield and quality of citrus fruits. Drought down-regulated the biosynthesis genes of auxin and gibberellin (YUC10, GA20OX1, GA2OX1, and GA20OX2) in fruits, up-regulated the decomposition gene of cytokinin (CKX5), and reduced the expression levels of plant hormone signal transduction-related genes (AUX/IAA, SAUR32, GH3.1, and ARRs), which may participate in the response of fruit size to drought stress. Meanwhile, drought treatment up-regulated the genes related to citric acid synthesis (PEPC2 and PEPCK1) and citric acid transport (PH1, PH4, PH8, and VHA-c3), which may regulate the accumulation of organic acids. Moderate water control during cultivation can enhance fruit quality, whereas severe drought may result in diminished yield and quality in citrus production. This study analyzed the effects of water regulation on citrus fruit expansion and citric acid accumulation at the transcriptomic level; future work will integrate metabolomics and physiological–biochemical analyses to systematically investigate the dynamic changes in endogenous hormone metabolism and the response patterns of key regulatory enzyme activities.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/horticulturae12070818/s1, Table S1. Primer sequences used for qRT-PCR; Table S2. Transcriptome sequencing information; Table S3. Gene list for Venn diagram; Table S4. List of all genes identified by transcriptome analysis; Table S5. Differentially expressed genes across water deficit treatments; Table S6. List of all genes in GO enrichment analysis; Table S7. KEGG enrichment analysis gradient table; Table S8. Genes related to the size of citrus fruits and the metabolism of citric acid; Figure S1. Correlation analysis between transcriptome FPKM values of differentially expressed genes and qRT-PCR results.

Author Contributions

Conceptualization, L.J. and P.W.; methodology, L.J. and L.P.; investigation, Y.W., Y.S. and F.L.; writing—original draft preparation, L.J.; writing—review and editing, L.J. and P.W.; supervision, P.W.; funding acquisition, L.J. and L.P. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by the National Natural Science Foundation of China (32202407) and the Taizhou Science and Technology Project (20ny17).

Data Availability Statement

The raw data of RNA-Seq have been uploaded to the China National Center for Bioinformation (CNCB, https://ngdc.cncb.ac.cn/gsa/, accessed on 12 March 2026). The accession number is CRA039788.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Aslan, M.N.; Sukan-Karaçağıl, B.; Acar-Tek, N. Roles of citrus fruits on energy expenditure, body weight management, and metabolic biomarkers: A comprehensive review. Nutr. Rev. 2024, 82, 1292–1307. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Dahro, B.; Li, C.; Liu, J.H. Overlapping responses to multiple abiotic stresses in citrus: From mechanism understanding to genetic improvement. Hortic. Adv. 2023, 1, 4. [Google Scholar] [CrossRef] [Scilit]
  3. Ma, X.; Sheng, L.; Li, F.; Zhou, T.; Guo, J.; Chang, Y.; Yang, J.; Jin, Y.; Chen, Y.; Lu, X. Seasonal drought promotes citrate accumulation in citrus fruit through the CsABF3-activated CsAN1-CsPH8 pathway. New Phytol. 2024, 242, 1131–1145. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Khan, M.A.; Zaman, F.; Liu, Y.; Alam, S.M.; Liu, D.; Han, H.; Luo, Y. Citrus NAC47 Modulates Vacuolar Storage of Soluble Sugars by Interacting With Type I H+-Pyrophosphatase Genes Under Drought Stress. Physiol. Plant. 2025, 177, e70303. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Khan, M.A.; Zaman, F.; Liu, Y.; Alam, S.M.; Han, H.; Luo, Y.; Ateeq, M. CsMYB1-CwINV6 Module Involves in the Promotion of Soluble Sugar Accumulation in Citrus Fruits Under Drought Stress. Plant Cell Environ. 2025, 48, 5572–5583. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Rahmati, M.; Vercambre, G.; Davarynejad, G.; Bannayan, M.; Azizi, M.; Génard, M. Water scarcity conditions affect peach fruit size and polyphenol contents more severely than other fruit quality traits. J. Sci. Food. Agric. 2015, 95, 1055–1065. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Lin, Q.; Qian, J.; Zhao, C.; Wang, D.; Liu, C.; Wang, Z.; Sun, C.; Chen, K. Low Temperature Induced Changes in Citrate Metabolism in Ponkan (Citrus reticulata Blanco cv. Ponkan) Fruit during Maturation. PLoS ONE 2016, 11, e156703. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  8. Ke, F.; Huang, X.; Sun, L.; Wang, L.; Nie, Z.; Yang, Y.; Cui, C. Integrating Transcriptomics and Metabolomics Analyses to Reveal the Potential Molecular Mechanism of Citrus junos Aroma Enhancement by Protected Cultivation. Horticulturae 2025, 11, 945. [Google Scholar] [CrossRef] [Scilit]
  9. Zhang, L.; Xu, Y.; Li, Y.; Zheng, S.; Zhao, Z.; Chen, M.; Yang, H.; Yi, H.; Wu, J. Transcription factor CsMYB77 negatively regulates fruit ripening and fruit size in citrus. Plant Physiol. 2024, 194, 867–883. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  10. Liu, C.; Li, D.; Huang, X.; Zhang, F.; Xie, Z.; Zhang, H.; Liu, J. Manual thinning increases fruit size and sugar content of Citrus reticulata Blanco and affects hormone synthesis and sugar transporter activity. J. Integr. Agric. 2022, 21, 725–735. [Google Scholar] [CrossRef] [Scilit]
  11. Kaneko, T.; Gould, N.; Campbell, D.; Clearwater, M.J. Isohydric stomatal behaviour alters fruit vascular flows and minimizes fruit size reductions in drought-stressed ‘Hass’ avocado (Persea americana Mill.). Ann. Bot. 2024, 133, 969–982. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Bu, H.; Yu, W.; Yuan, H.; Yue, P.; Wei, Y.; Wang, A. Endogenous Auxin Content Contributes to Larger Size of Apple Fruit. Front. Plant Sci. 2020, 11, 592540. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Bu, H.; Sun, X.; Hu, Y.; Gu, G.; Yang, Y.; Yu, W. Research Advances in the Regulation of Fruit Size: An Integrated Perspective of Genetic, Hormonal, Epigenetic, and Environmental Control. Biology 2025, 14, 1643. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Gonzalez, N.; Gévaudant, F.; Hernould, M.; Chevalier, C.; Mouras, A. The cell cycle-associated protein kinase WEE1 regulates cell size in relation to endoreduplication in developing tomato fruit. Plant J. 2007, 51, 642–655. [Google Scholar] [PubMed]
  15. Boonkorkaew, P.; Hikosaka, S.; Sugiyama, N. Effect of pollination on cell division, cell enlargement, and endogenous hormones in fruit development in a gynoecious cucumber. Sci. Hortic. 2008, 116, 7. [Google Scholar] [CrossRef] [Scilit]
  16. Naor, A. Irrigation and Crop Load Influence Fruit Size and Water Relations in Field-grown ‘Spadona’ Pear. J. Am. Soc. Hortic. Sci. 2001, 126, 252–255. [Google Scholar] [CrossRef] [Scilit]
  17. Thu, A.M.; Alam, S.M.; Khan, M.A.; Han, H.; Liu, D.; Tahir, R.; Ateeq, M.; Liu, Y. Foliar spraying of potassium sulfate during fruit development comprehensively improves the quality of citrus fruits. Sci. Hortic. 2024, 338, 113696. [Google Scholar] [CrossRef] [Scilit]
  18. Lu, X.; Cao, X.; Li, F.; Li, J.; Xiong, J.; Long, G.; Cao, S.; Xie, S. Comparative transcriptome analysis reveals a global insight into molecular processes regulating citrate accumulation in sweet orange (Citrus sinensis). Physiol. Plant. 2016, 158, 463–482. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Hussain, S.B.; Shi, C.; Guo, L.; Kamran, H.M.; Sadka, A.; Liu, Y. Recent Advances in the Regulation of Citric Acid Metabolism in Citrus Fruit. Crit. Rev. Plant Sci. 2017, 36, 241–256. [Google Scholar] [CrossRef] [Scilit]
  20. Guo, L.; Liu, Y.; Luo, L.; Hussain, S.B.; Bai, Y.; Alam, S.M. Comparative Metabolites and Citrate-Degrading Enzymes Activities in Citrus Fruits Reveal the Role of Balance between ACL and Cyt-ACO in Metabolite Conversions. Plants 2020, 9, 350. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Li, S.; Yin, X.; Wang, W.; Liu, X.; Zhang, B.; Chen, K. Citrus CitNAC62 cooperates with CitWRKY1 to participate in citric acid degradation via up-regulation of CitAco3. J. Exp. Bot. 2017, 68, 3419–3426. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Jin, L.; Yue, Y.; Liu, F.; Wen, M.; Huang, B.; Wang, P. Identification of the Grapefruit (Citrus paradisi) Isocitrate Dehydrogenase Gene and Functional Analysis of CpNADP-IDH1 in Citric Acid Metabolism. Horticulturae 2025, 11, 598. [Google Scholar] [CrossRef] [Scilit]
  23. Jin, L.; Wen, M.; Liu, F.; Huang, B.; Wang, P. Physiological and Transcriptomic Analysis of Citrus Fruit Segment Drying under Facility-Forcing Cultivation. Horticulturae 2024, 10, 807. [Google Scholar] [CrossRef] [Scilit]
  24. Jin, L.; Yin, X.; Wen, M.; Huang, B.; Liu, F.; Li, X.; Wang, P. Genome-Wide Identification, Characterization, and Expression of the HAK/KUP/KT Potassium Transporter Gene Family in Poncirus trifoliata and Functional Analysis of PtKUP10 under Salt Stress. Horticulturae 2024, 6, 628. [Google Scholar]
  25. Tie, Z.; Bin, P.; Feifei, L.; Xiaochuan, M.; Mengjing, T.; Xuefei, L.; Yuanyuan, C.; Yuewen, C.; Xiaopeng, L. Effects of drought stress at enlargement stage on fruit quality formation of Satsuma mandarin and the law of water absorption and transportation in tree after re-watering. Acta Hortic. Sin. 2022, 49, 11–22. [Google Scholar]
  26. Navarro, J.M.; Pérez-Pérez, J.G.; Romero, P.; Botía, P. Analysis of the changes in quality in mandarin fruit, produced by deficit irrigation treatments. Food Chem. 2010, 119, 1591–1596. [Google Scholar] [CrossRef] [Scilit]
  27. Jiang, N.; Jin, L.; Teixeira Da Silva, J.A.; Islam, M.Z.; Gao, H.; Liu, Y.; Peng, S. Activities of enzymes directly related with sucrose and citric acid metabolism in citrus fruit in response to soil plastic film mulch. Sci. Hortic. 2014, 168, 73–80. [Google Scholar] [CrossRef] [Scilit]
  28. Ji, J.; Yang, L.; Fang, Z.; Zhang, Y.; Zhuang, M.; Lv, H.; Wang, Y. Plant SWEET Family of Sugar Transporters: Structure, Evolution and Biological Functions. Biomolecules 2022, 12, 205. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Feng, G.; Wu, J.; Xu, Y.; Lu, L.; Yi, H. High-spatiotemporal-resolution transcriptomes provide insights into fruit development and ripening in Citrus sinensis. Plant Biotechnol. J. 2021, 19, 1337–1353. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Mauxion, J.; Chevalier, C.; Gonzalez, N. Complex cellular and molecular events determining fruit size. Trends Plant Sci. 2021, 26, 1023–1038. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Pandolfini, T.; Molesini, B.; Spena, A. Molecular dissection of the role of auxin in fruit initiation. Trends Plant Sci. 2007, 12, 327–329. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Fenn, M.A.; Giovannoni, J.J. Phytohormones in fruit development and maturation. Plant J. 2021, 105, 446–458. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Cruz-Castillo, J.G.; Woolley, D.J.; Lawes, G.S. Kiwifruit size and CPPU response are influenced by the time of anthesis. Sci. Hortic. 2002, 95, 23–30. [Google Scholar] [CrossRef] [Scilit]
  34. Zhao, X.; Zhao, Z.; Cheng, S.; Wang, L.; Luo, Z.; Ai, C.; Liu, Z.; Liu, P.; Wang, L.; Wang, J.; et al. ZjWRKY23 and ZjWRKY40 Promote Fruit Size Enlargement by Targeting and Downregulating Cytokinin Oxidase/Dehydrogenase 5 Expression in Chinese Jujube. J. Agric. Food. Chem. 2023, 71, 18046–18058. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Le, D.T.; Ha, C.V.; Nguyen, K.H.; Chu, H.D.; Zhu, C.; Li, W.; Watanabe, Y.; Kojima, M.; Takebayashi, Y.; Sakakibara, H. Altering endogenous cytokinin content by GmCKX13 as a strategy to develop drought-tolerant plants. Plant Stress 2024, 14, 100678. [Google Scholar]
  36. Jia, D.; Xu, Z.; Chen, L.; Huang, Q.; Huang, C.; Tao, J.; Qu, X.; Xu, X. Analysis of organic acid metabolism reveals citric acid and malic acid play major roles in determining acid quality during the development of kiwifruit (Actinidia eriantha). J. Sci. Food. Agric. 2023, 103, 6055–6069. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Shi, C.; Song, R.; Hu, X.; Liu, X.; Jin, L.; Liu, Y. Citrus PH5-like H+-ATPase genes: Identification and transcript analysis to investigate their possible relationship with citrate accumulation in fruits. Front. Plant Sci. 2015, 6, 135. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Shi, C.; Hussain, S.B.; Guo, L.; Yang, H.; Ning, D.; Liu, Y. Genome-wide identification and transcript analysis of vacuolar-ATPase genes in citrus reveal their possible involvement in citrate accumulation. Phytochemistry 2018, 155, 147–154. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Shi, C.; Hussain, S.B.; Han, H.; Alam, S.M.; Liu, D.; Liu, Y. Reduced expression of CsPH8, a P-type ATPase gene, is the major factor leading to the low citrate accumulation in citrus leaves. Plant Physiol. Biochem. 2021, 160, 211–217. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. Wu, K.; Hu, C.; Duan, Y.; Moussa, M.G.; Li, J.; Lou, W.; Sun, X.; Yan, X.; Tan, Q.; Wu, S. Potassium Promotes Citric Acid Accumulation by Regulating Its Synthesis and Vacuole Storage in Newhall Navel Orange (Citrus sinensis). J. Agric. Food. Chem. 2025, 73, 12072–12082. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  41. Lu, C.; Lu, Y.; Zhao, Y. Overexpression of the GsPPC4 gene from Gleditsia sinensis enhances low phosphate tolerance in tobacco by promoting organic acid secretion. Biochem. Biophys. Res. Commun. 2025, 779, 152426. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. The transverse section of normal (CK), moderate drought (MD), and severe drought (SD) fruit. The white line is 2 cm.
Horticulturae 12 00818 g001
Figure 2. Transcriptome analysis among normal (CK), moderate drought (MD), and severe drought (SD) fruits. (A) PCA. (B) Screening different expression genes among SD, MD, and CK fruits. (C) Venn diagram of differently expressed genes among SD, MD, and CK fruits.
Horticulturae 12 00818 g002
Figure 3. GO enrich analysis of different expression genes among normal (CK), moderate drought (MD), and severe drought (SD) fruits.
Horticulturae 12 00818 g003
Figure 4. KEGG enrichment analysis of differentially expressed genes among normal (CK), moderate drought (MD), and severe drought (SD) fruits. (A) CK-vs-MD, (B) CK-vs-SD, (C) MD-vs-SD.
Horticulturae 12 00818 g004
Figure 6. qRT-PCR validation of the different expression genes. All data are shown as mean ± standard error (n = 3). Different lowercase letters indicate significant differences (p < 0.05).
Horticulturae 12 00818 g006
Table 1. The quality parameters of normal (CK), moderate drought (MD), and severe drought (SD) fruit. L: lightness, a: red/green axis, b: yellow/blue axis, FW: fruit weight, LD: longitudinal diameter, TD: transverse diameter, TSS: total soluble solids, TA: titratable acidity, CA: citric acid content. All data are shown as mean ± standard error (n = 9). Different lowercase letters indicate significant differences (p < 0.05).
LabFW (g)LD (mm)TD (mm)TSS (%)TA (mg/100 mL)CA
(mg/g)
TARVc (mg/100 mL)
CK73.1 ± 2.1 b0.4 ± 1.9 a71.1 ± 2.3 a177.4 ± 18.5 a73.9 ± 7.8 a82.1 ± 5.6 a12.5 ± 0.8 c1.0 ± 0.1 c46.3 ± 1.0 a12.9 ± 1.2 a31.3 ± 5.3 b
MD76.9 ± 0.7 a−1.8 ± 1.0 a68.2 ± 2.3 b189.1 ± 41.8 a78.9 ± 10.8 a74.5 ± 5.4 b16.6 ± 1.3 b2.8 ± 0.4 b25.1 ± 0.3 b5.9 ± 0.6 b31.7 ± 5.3 b
SD77.5 ± 3.1 a−0.4 ± 4.0 a70.51 ± 2.9 ab60.1 ± 10.7 b51.1 ± 3.8 b49.2 ± 2.9 c20.4 ± 1.5 a4.2 ± 1.4 a8.9 ± 1.0 c5.3 ± 1.4 b39.8 ± 5.6 a
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.