Review

Virus-Induced Gene Silencing (VIGS) in Functional Genomics: Advances and Applications in Capsicum annuum L.


1
All-Russian Research Institute of Agricultural Biotechnology (FSBSI ARRIAB), 127550 Moscow, Russia
2
Federal Research Center of Biological Plant Protection (FSBSI FRCBPP), 350039 Krasnodar, Russia
*
Author to whom correspondence should be addressed.
Horticulturae 2025, 11(11), 1297; https://doi.org/10.3390/horticulturae11111297
Submission received: 10 September 2025 / Revised: 14 October 2025 / Accepted: 18 October 2025 / Published: 29 October 2025
(This article belongs to the Special Issue Genetics, Genomics and Breeding of Vegetable Crops)

Abstract

This article provides a comprehensive analysis of Virus-Induced Gene Silencing (VIGS), which is an effective tool for studying the functional genomics of organisms that are poorly amenable to genomic editing. The VIGS method is grounded in the plant’s post-transcriptional gene silencing (PTGS) machinery and utilizes recombinant viral vectors to trigger systemic suppression of endogenous plant gene expression, leading to visible phenotypic changes that enable gene function characterization. This article details the application of VIGS in model organisms (Arabidopsis thaliana, Nicotiana benthamiana) and a wide range of crops, with a special focus on the Solanaceae family, particularly pepper (Capsicum annuum L.). This review analyzes the design and structural elements of viral vectors used for VIGS, such as Tobacco Rattle Virus (TRV), Broad Bean Wilt Virus 2 (BBWV2), Cucumber Mosaic Virus (CMV), geminiviruses (CLCrV, ACMV), and satellite virus-based systems. It also critically examines the key factors that determine silencing efficiency. These factors encompass insert design, agroinfiltration methodology, plant developmental stage, agroinoculum concentration, plant genotype, and environmental factors (temperature, humidity, photoperiod). Particular attention is given to optimization strategies, such as the use of viral suppressors of RNA silencing (VSRs). This article concludes with the achievements in using VIGS to identify pepper genes governing fruit quality (color, biochemical composition, pungency), resistance to biotic (bacteria, oomycetes, insects) and abiotic (temperature, salt, osmotic stress) factors, as well as genes regulating plant architecture and development. The results obtained demonstrate the advantages and limitations of VIGS, alongside future perspectives for its integration with multi-omics technologies to accelerate breeding and advance functional genomics studies in pepper.

1. Introduction

Studying gene function is a central task in molecular biology, providing the foundational knowledge required for modern plant breeding and genetic engineering. This field, known as functional genomics, aims to understand not only the structure of genomes but also the dynamic processes of gene expression, regulation, and interaction.
Advances in sequencing technologies have led to an explosion of genomic data for a wide range of plant species, from compact genomes to those exceeding 10 Gb [1]. However, sequencing alone reveals the blueprint of an organism without explaining the biological functions of its genes. While powerful genome-editing techniques like CRISPR/Cas9 [2], TALEN [3] and ZFN [4], as well as mutagenesis-based approaches [5,6,7], exist for functional characterization, they are often labor-intensive, costly, and reliant on stable transformation [8,9]. Virus-induced gene silencing (VIGS) has emerged as a potent and flexible alternative that bypasses these limitations [9]. As a transient, sequence-specific post-transcriptional gene silencing method, VIGS offers a faster and less expensive means of linking genes to functions, contributing to its widespread adoption [8].
The foundation of VIGS was laid in 1995 when Kumagai et al. used a Tobacco mosaic virus vector carrying a fragment of the phytoene desaturase (PDS) gene from Nicotiana benthamiana to induce silencing, resulting in a characteristic photo-bleaching phenotype [10]. This pioneering work established VIGS as a powerful genetic tool, which has since been adapted for use in a diverse array of plant species, including woody plants [11,12].
Since its initial demonstration, the VIGS toolkit has expanded significantly. The development of vectors based on various viruses, such as Alfalfa mosaic virus (AMV) [13], and Cotton leaf crumple virus (CLCrV) [14], has broadened the range of amenable host plants. To date, VIGS has been successfully applied for functional gene analysis in over 50 plant species, including major crops like tomato [15], barley [16], soybean [17], and cotton [18], enabling the characterization of hundreds of genes involved in disease resistance, abiotic stress responses, and metabolism [8,19]. Among these, TRV-based vectors have emerged as particularly versatile tools due to their broad host range, efficient systemic movement, and ability to target meristematic tissues, making them one of the most widely adopted VIGS systems across diverse plant families [20,21,22].
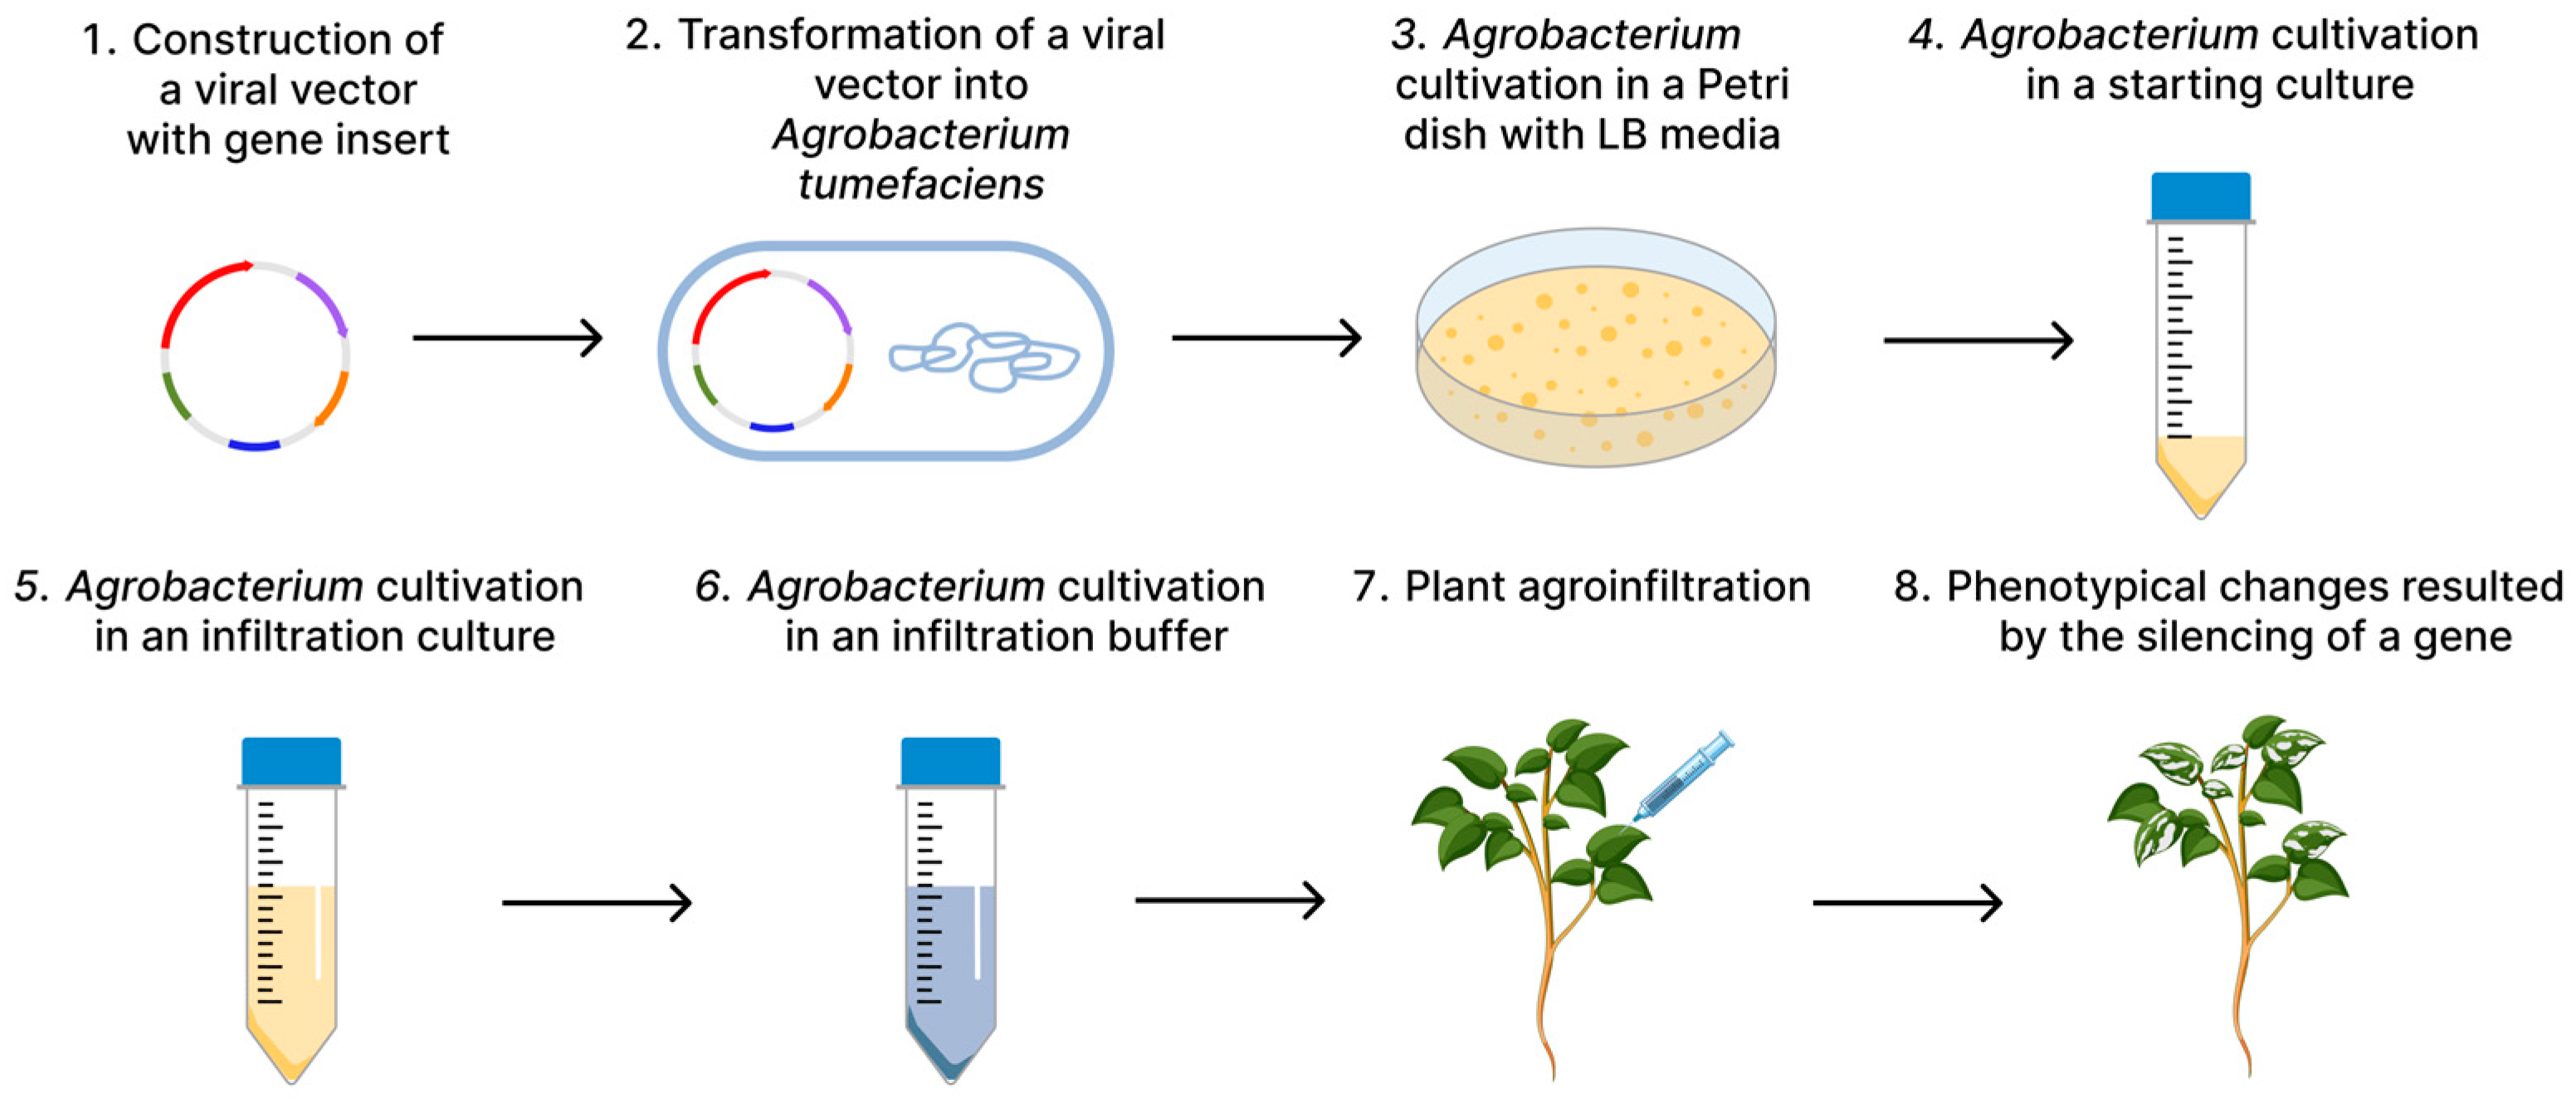
The biological basis of VIGS is the mechanism of post-transcriptional gene silencing (PTGS) [8]. This mechanism is employed by plants as an antiviral defense system. The PTGS mechanism involves the cleavage of long double-stranded RNA (dsRNA)—a common replication intermediate for many viruses. This processing is mediated by cellular Dicer-like enzymes (DCL), generating 21- to 24-nucleotide small interfering RNAs (siRNAs). These siRNAs are then incorporated into an RNA-induced silencing complex (RISC), which guides the sequence-specific degradation of complementary viral mRNA, thereby suppressing infection. It is crucial to distinguish these virus-derived siRNAs from endogenous microRNAs (miRNAs), which are processed from distinct, endogenous stem-loop precursor transcripts and primarily regulate plant development. The fundamental principles of PTGS are detailed in the works of Zulfiqar et al. [8] and Wieczorek et al. [23]. A schematic representation of VIGS technology is shown in Figure 1.
While VIGS is highly efficient in model plants like Arabidopsis thaliana [24,25] and Nicotiana benthamiana [26,27] due to their small genomes and rapid life cycles [28], its application in non-model crops presents significant challenges. This is particularly true for vegetable pepper (Capsicum annuum L.), a species renowned for its high genetic diversity and complex biochemistry, including unique capsaicinoid biosynthesis pathways [29,30,31,32,33,34]. Furthermore, its genome contains extensive families of functionally redundant genes, complicating the interpretation of silencing phenotypes. Stable genetic transformation of pepper remains difficult and genotype-dependent due to low regeneration efficiency, making VIGS not merely a convenient alternative but often the key, and sometimes the only viable tool for high-throughput functional screening in this crop [35,36].
The effectiveness of VIGS is influenced by a multitude of factors, including the molecular characteristics of the host plant [37,38,39]. For instance, Argonaute proteins, which are central to the RNA interference machinery, can vary significantly between plant species [37,38]. Furthermore, the intercellular and long-distance movement of siRNAs, which is essential for the systemic propagation of silencing signals, exhibits species-specific variation, consequently influencing the overall efficiency of VIGS [39]. Another critical layer of complexity arises from viral counter-defenses. To overcome the plant’s post-transcriptional silencing mechanisms, many viruses have evolved viral suppressors of RNA silencing (VSRs) that inhibit host defenses [23,40,41,42]. Research has demonstrated that the efficacy of these suppressors varies among plant species, a consideration exploited to enhance VIGS efficiency, for example, through the use of well-characterized VSRs like P19 and C2b [40].
This review synthesizes advances in the application of Virus-Induced Gene Silencing (VIGS) technology for the functional genomics of Solanaceae plants, with a special focus on vegetable pepper (Capsicum annuum L.). It provides a critical analysis of the key factors determining silencing efficiency, including vector optimization, the design of genetic constructs, and strategies for employing viral suppressors of RNA silencing (VSRs) to enhance the method’s efficacy. Particular attention is given to the practical aspects of VIGS implementation, specifically the influence of cultivation conditions (temperature, humidity, photoperiod), inoculation parameters (agrobacterial optical density, delivery method), and plant genotypic specificities on the success of target gene knockdown. The review details the achievements in using VIGS to identify genes controlling agronomically valuable traits in pepper, such as pathogen resistance, abiotic stress tolerance, and unique metabolic pathways. Finally, this article discusses future perspectives for the technology, including the development of combinatorial screening platforms and the potential of VIGS as a tool for accelerated crop breeding.

2. Viral Vectors Used in VIGS

Currently, at least 50 viral vectors of various types, capable of infecting both dicotyledonous and monocotyledonous plants, are used in VIGS [8,43]. Viral vectors serve to deliver nucleotide sequences of genes into plants, leading to their knockdown via post-transcriptional silencing [8,44]. Viral vectors are categorized into DNA viruses, RNA viruses, and vectors based on satellite viruses [14,45,46,47,48]. The constructs of viral vectors of different natures differ from each other in genome composition, duration of effect, and the induction of symptoms in the plant.
In this article, we have outlined the key viral vectors used in VIGS technology, with an emphasis on their structural features. For a more visual comparison of a broader spectrum of vectors, which includes their origin, advantages, limitations, and host-specific applications, we direct the reader to specialized review articles where this information is systematized in comparative tables [19,43,49,50].

2.1. Vectors Based on RNA Viruses

Vectors based on RNA viruses are characterized by cytoplasmic localization of replication, which is carried out by a specific virus-encoded RNA-dependent RNA polymerase (RdRp). When using agroinfiltration methods, the initial transcription of viral sequences integrated into plasmid vectors occurs in the nucleus with the participation of host RNA polymerase II. Advantages of RNA vectors include their relatively low molecular weight, which promotes efficient systemic spread, and high efficiency of gene suppression, achieved within a short time after inoculation. A significant drawback of many RNA vectors is the induction of pronounced viral infection symptoms, which can complicate the interpretation of phenotypic data [48,51,52].

2.1.1. Tobacco Rattle Virus (TRV)

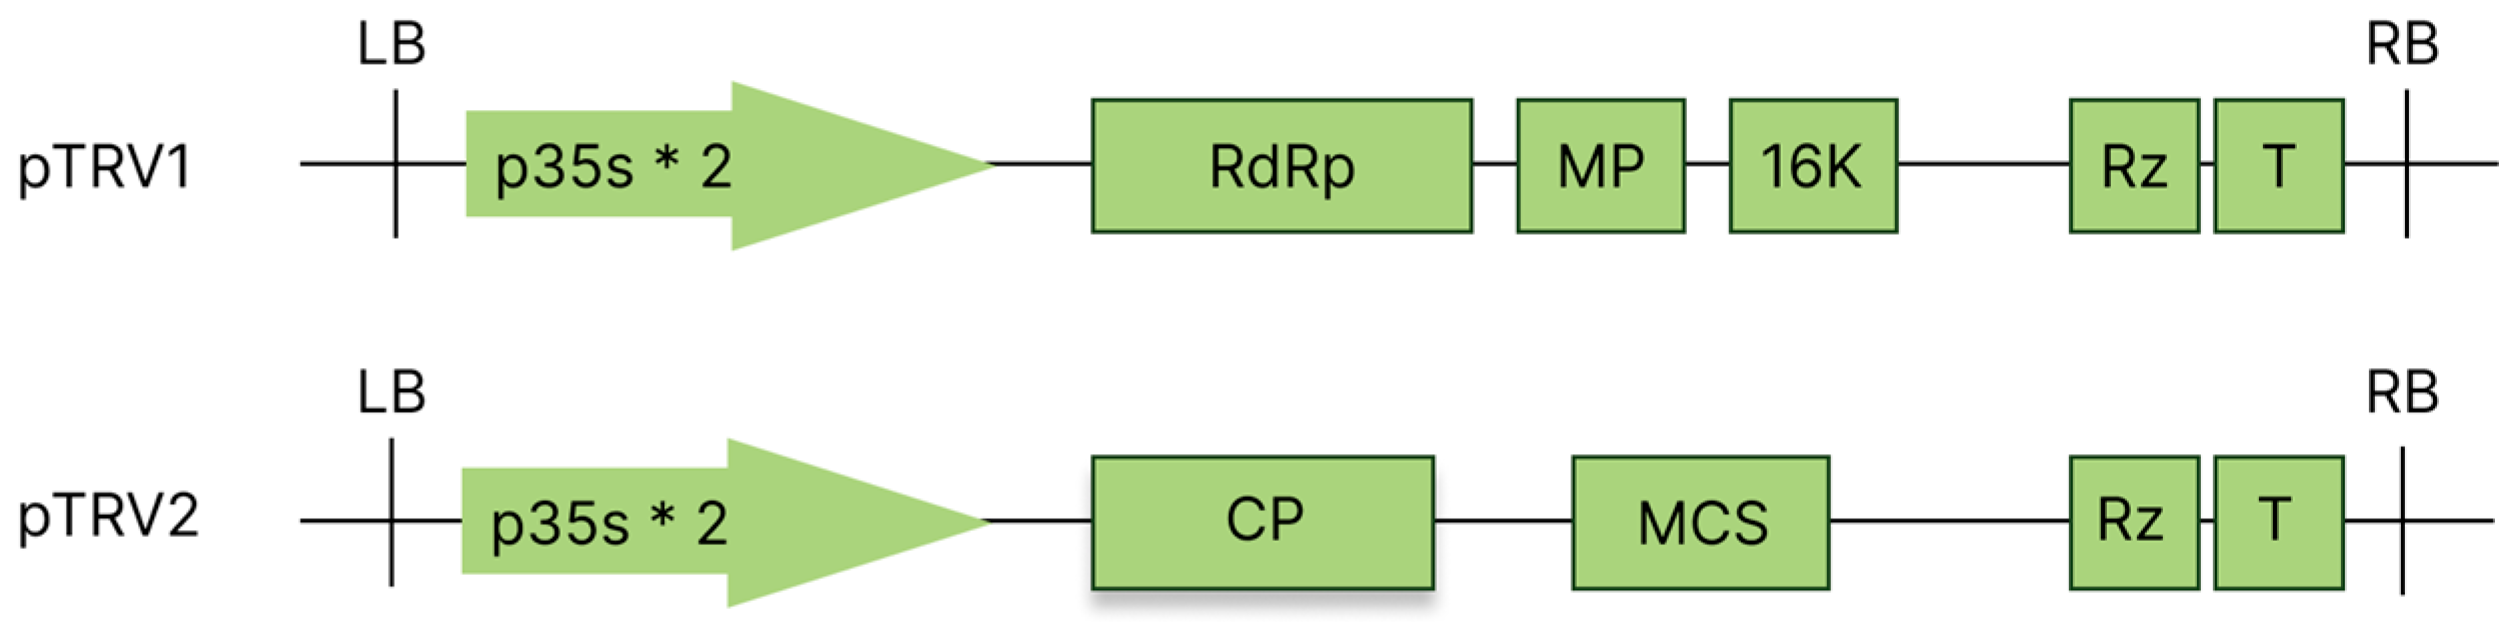
The vector based on Tobacco rattle virus (TRV) is one of the most versatile and widely used systems for VIGS, especially for plants of the Solanaceae family. The bipartite genome organization of TRV requires the use of two vectors: TRV1 and TRV2. The TRV1 plasmid construction encodes replicase proteins (134 and 194 kDa), a movement protein (29 kDa), and a weak RNA interference suppressor (16 kDa), ensuring virus replication and systemic spread. TRV2 contains the capsid protein gene and a multiple cloning site for inserting target sequences, playing a key role in initiating silencing [20,21,53]. Both vectors typically contain a self-cleaving ribozyme sequence to ensure correct transcript processing. The schematic structure of the TRV vectors is shown in Figure 2.
Key advantages of the TRV system are high silencing efficiency, long duration of action, a broad range of host plants, and minimal severity of viral symptoms [20,21,22]. The compact genome size facilitates cloning and agroinfiltration processes, and the lack of integration into the host plant’s genome minimizes the risks of mutagenesis [54].
Of particular importance is TRV ability to infect apical meristems and actively dividing tissues [21]. Unlike many other viral vectors, which are effectively excluded from meristematic zones, TRV overcomes this barrier, allowing for the study of genes involved in development and cell division. This unique feature, combined with efficient systemic spread via phloem transport, ensures deep and stable silencing of targets in various plant tissues.
An important feature of the system is the possibility of its further modification. To enhance silencing efficiency, genes for viral suppressors of RNA silencing (VSR) that suppress the host plant’s defense mechanisms can be incorporated into the vector construct [55]. Furthermore, modification of vectors using the green fluorescent protein (GFP) gene is widely used for visual monitoring of the infection process, allowing for real-time tracking of virus spread in plant tissues [56].
Phenotypic manifestations of silencing usually develop within an interval of 7 to 35 days after infiltration, depending on the plant species [15,18,36,56,57,58,59,60]. TRV demonstrates high efficiency on various crops of the Solanaceae family, including tomato [15], potato [60], eggplant [57], and pepper [36], as well as on some monocot species. However, silencing efficiency may decrease in non-solanaceous representatives [56], necessitating the use of alternative vector systems for certain plant groups.

2.1.2. Other Vectors Based on RNA Viruses

Other vector systems have been developed for solving specialized tasks. A promising development for plants of the Solanaceae family is the system based on Broad bean wilt virus 2 (BBWV2). In the study by Boram Choi et al., the BBWV2-R2 vector was developed, which causes systemic infection in pepper without pronounced symptoms [45]. The vector design involves a tandem insertion of genetic sequences between the MP and LCP cistrons using BglII and AvrII restriction sites. This approach allows for simultaneous expression of two genes in the same cells. To enhance the expression of recombinant proteins, heterologous viral suppressors of RNA silencing (VSR) from a dual BBWV2-based vector are co-expressed in the system (Figure 3).
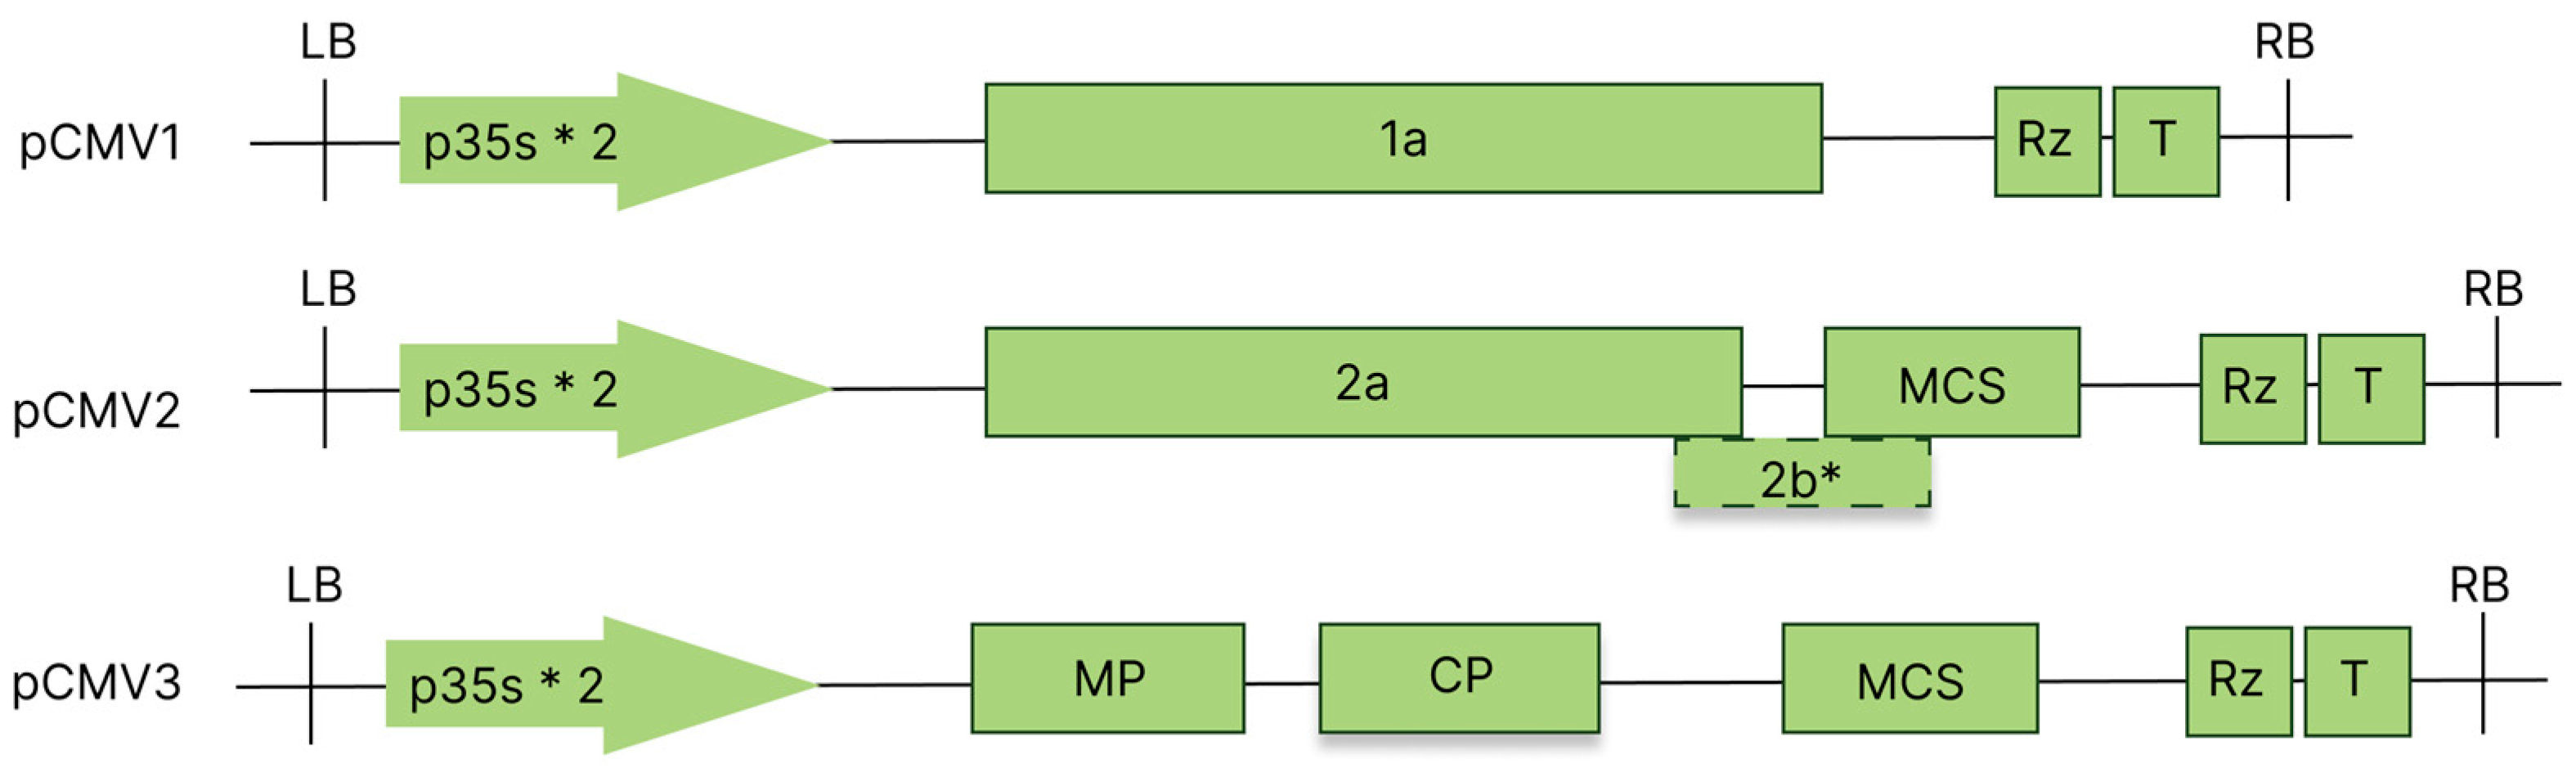
Another promising system for functional studies of genes in Solanaceae crops is the vector based on Cucumber mosaic virus (CMV). The compact genome size and wide host range make this system particularly convenient for comparative studies [46,61]. The tripartite genome organization of CMV includes vectors pCMV1, pCMV2, and pCMV3. pCMV1 and pCMV2 encode proteins 1a and 2a, responsible for virus replication and formation of viral particles, respectively (Figure 4). The 2b protein, whose gene is located in pCMV2, functions as an RNA silencing suppressor [62,63]. pCMV3 contains the genes for the movement protein (MP) and the capsid protein (CP). Various modification strategies are used to create vectors: insertion of a multiple cloning site (MCS) into the deletion site of the 2b protein gene in pCMV2 [46,61,64] or addition of an MCS after the capsid protein gene in pCMV3. In the study by Liao et al. [65], a vector containing an integrated Target Mimic (TM) sequence was created based on this system. The TM sequence acts as a decoy for specific plant siRNAs and was inserted between the SpeI and MluI restriction sites in the MCS.

2.2. Vectors Based on DNA Viruses

Vectors based on DNA viruses (primarily geminiviruses) are characterized by nu-clear localization of their replication cycle. Initially, transcription of the vector genes, including the replication-associated protein (Rep), is carried out by the host plant’s RNA polymerase II [19]. Subsequently, the synthesized Rep protein initiates viral DNA replication via a rolling circle mechanism [66]. The main advantages of DNA vectors are the relative simplicity of the construct and stability. However, the larger genome size can limit the efficiency of systemic spread and silencing [19].
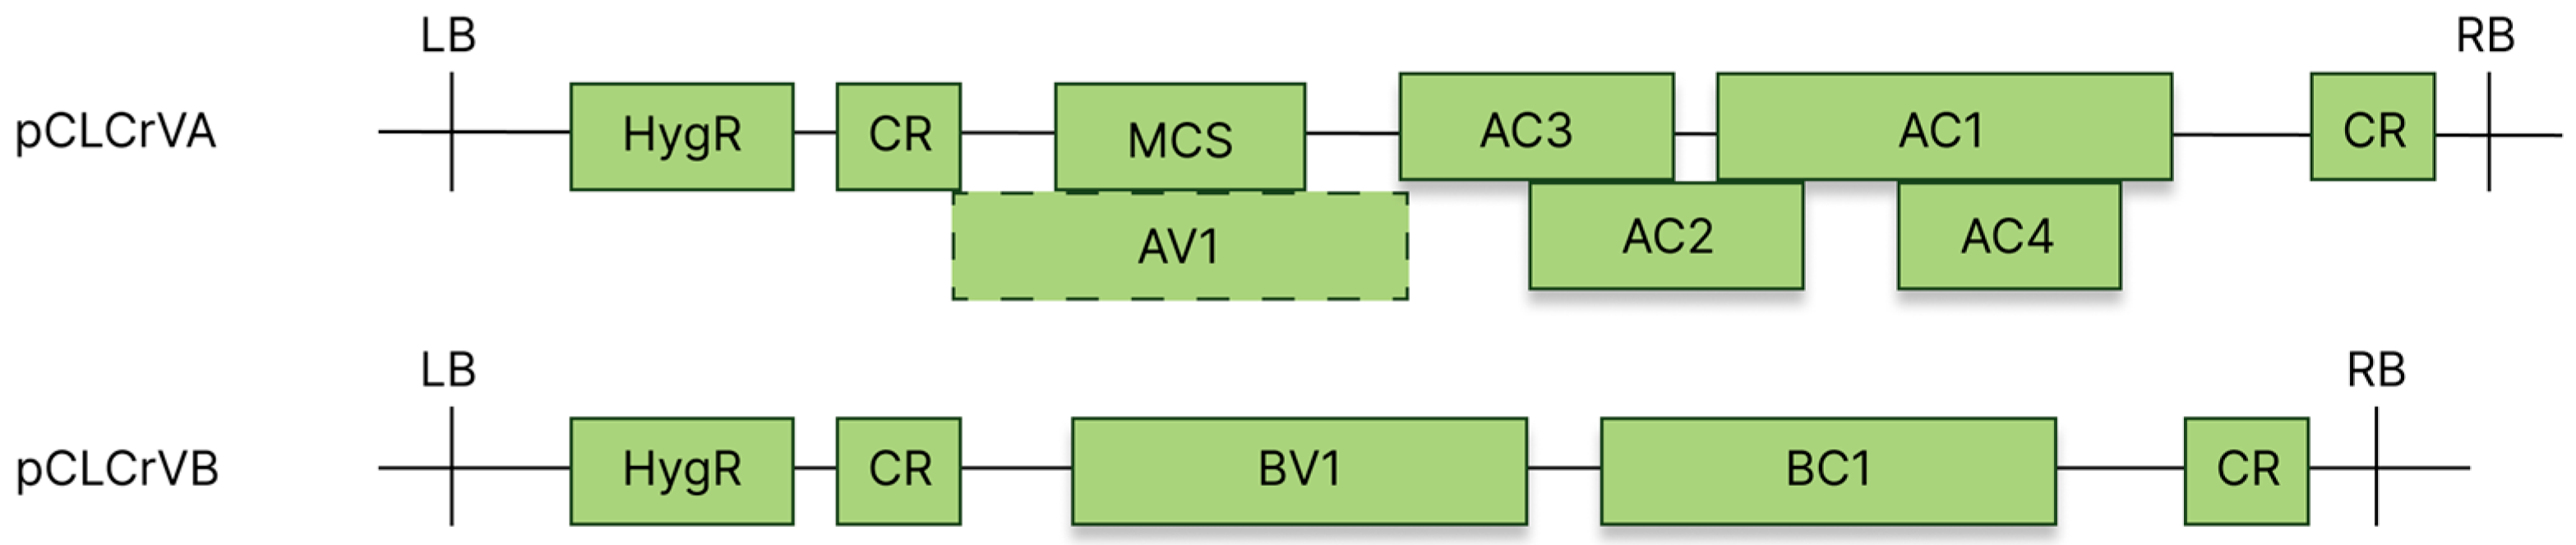
Cotton Leaf Crumple Virus (CLCrV). As an example of the DNA vectors used, a viral vector based on the cotton wrinkle virus (CLCrV) can be characterized. Two cDNA vectors are used for infection: DNA-A (pCLCrVA) and DNA-B (pCLCrVB). DNA-A (~2.6 kb) contains genes encoding coat protein (AV1), viral replication protein (AC1), transcription protein (AC2), and replication enhancer protein (AC3). DNA-B (~2.6 kb) contains genes encoding the nuclear protein (BV1) and the plasmodesmus transfer protein (BC1) [14,47]. When creating the vectors, a multiple cloning site (MCS) was inserted into the place of the AV1 gene in pCLCrVA. pCLCrVA and pCLCrVB also contain common region (CR) that encodes regulatory elements needed for viral replication and translation. Modern CLCrV vectors also contain the HygR gene responsible for resistance to the antibiotic hygromycin B [47] (Figure 5). CLCrV vectors are mainly used to study the genes of plants of the Malvaceae family, especially cotton (Gossypium) [14,47].
Another important example of a plant DNA virus used in VIGS is African cassava mosaic virus (ACMV), a member of the family Geminiviridae [67]. The efficacy of this viral vector stems from its nuclear replication capability, systemic movement, and strong capacity to induce RNA silencing. Its utility has been demonstrated in studies involving both model plants and the agriculturally important crop cassava [68,69].
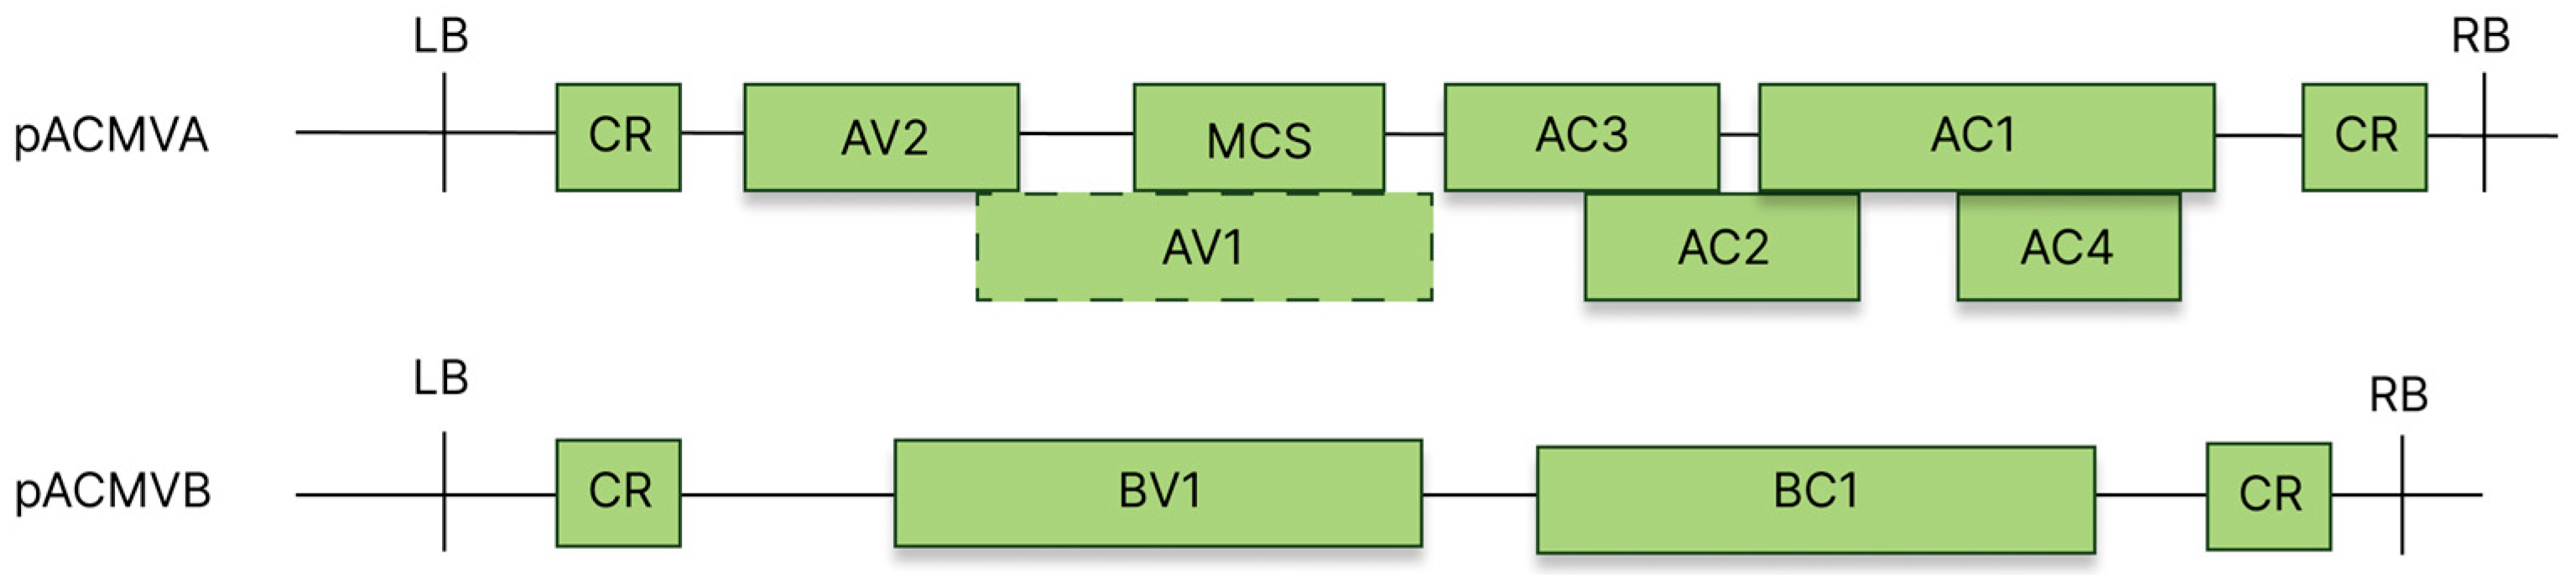
The structure of the ACMV vector also consists of two ring molecules: DNA-A pACMVA and DNA-B pACMVB with a length of ~2.8 kb. pACMVA contains the genes AC1 (Rep), AC2 (TrAP), AC3 (REn), AC4, AV1 (CP), AV2. All the genes are similar to their functional homologues in CLCrV, and the AC4 gene encodes a protein associated with the suppression of gene silencing. pACMVB contains the BC1 gene, encoding a nuclear protein, and the BV1 gene, a protein for moving the virus through the plasmodesmus [67,69]. The AV1 protein and AV2 protein encode coat protein (CP) and RNAi suppressor protein, respectively. Both ACMV vectors contain common regions of vector (CR), essential for viral replication and translation. Similarly, in the pACMVA vector, AV1 was replaced by a multiple cloning site into which the gene of interest can be inserted (Figure 6).

2.3. Satellite Systems Used in VIGS

Satellites are subviral agents whose replication and systemic spread completely depend on a helper virus. Depending on their ability to encode their own capsid protein, they are divided into satellite viruses and satellite RNAs. Due to their compact genome size and minimal pathogenic effects, both groups are of interest for the development of VIGS vectors [70,71,72].

2.3.1. Satellite Viruses (Using RNA-Containing Examples)

A classic example of an RNA satellite virus is the Satellite Tobacco Mosaic Virus (STMV), used as a vector in the SVISS (Satellite Virus-Induced Silencing System). In this system, developed by Gosselé et al., 2002 [71], STMV serves as the vector for delivering target sequences, while the Tobacco Mosaic Virus strain U2 (TMV-U2) acts as the helper virus, providing the replication and movement proteins. A key advantage of this approach is the separation of functions: the replication components are separated from the silencing-inducing components, which enhances system stability and silencing intensity.
To create the vector, the researchers used the infectious clone pSTMV10, in which a frameshift mutant pSTMVFS was generated in the capsid protein gene, incorporating an AgeI restriction site for inserting target gene fragments. The system demonstrated high efficiency in inducing knockdown of a wide range of endogenous genes, including genes involved in leaf and flower pigmentation (PDS, chsA), cell wall synthesis cesA-1a, cesA-2, as well as the ubiquitously expressed RNA polymerase II gene. Silencing phenotypes were pronounced and persisted for several weeks, and in the case of genes affecting plant growth, for up to 6 months. Effective silencing was achieved with insert lengths ranging from 100 to 300 nucleotides and was independent of insert orientation. Importantly, the system worked successfully not only with inoculation by in vitro transcripts but also using agroinfiltration with the pTVE334 construct containing the chimeric satellite virus in the T-DNA [71].

2.3.2. Helper-Dependent Satellite Vectors (DNA Betasatellites)

The most studied and practically significant representatives of satellite nucleic acids are DNA betasatellites of geminiviruses. It is important to note that in strict taxonomy, these agents are not full-fledged viruses, as they do not encode their own capsid protein and depend on a helper virus not only for replication but also for packaging and systemic movement [70]. This is precisely how they differ from true satellite viruses.
A prominent example of such a system is an optimized vector based on the betasatellite of Tomato yellow leaf curl China virus (TYLCCNV). In the work of Ju et al., 2017, the p1.7A+2mβ vector was developed, in which the pathogenicity gene βC1 was replaced by a multiple cloning site [70]. This construct, containing both the modified satellite (2mβ) and the helper virus genome (1.7A DNA-A) in a single T-DNA, demonstrated not only highly efficient knockdown of the endogenous PDS gene at the post-transcriptional level (VIGS) but also, crucially, successfully induced virus-induced transcriptional gene silencing (VITGS) of a GFP transgene. This was achieved by delivering a fragment of the 35S promoter, which led to heritable cytosine methylation in CG, CHG, and CHH contexts and stable promoter shutdown. Important advantages of this vector are its nuclear localization, minimal viral symptoms, and ability to induce epigenetic modifications, making it a powerful tool for functional studies beyond classical VIGS.

3. Factors Affecting the Effectiveness of VIGS

The outcome of the VIGS experiment is influenced by a wide range of factors. Obtaining reliable results of plant gene suppression requires proper implementation of all stages of VIGS. These stages include the creation of a viral vector design and insertion [47,55,73,74], the selection of the plant growth stage [17,35,75] the method of vector inoculation [76,77,78,79], and the control of abiotic growth conditions [35,80,81,82,83,84].

3.1. Viral Suppressors of RNA Silencing

A substantial body of knowledge has been accumulated regarding the interactions between pathogens and their host plants, including molecular mechanisms described by the “gene-for-gene” concept. Most plant viruses have evolved strategies to overcome the host’s RNA interference defense mechanism [85]. These strategies include encoding specialized proteins known as viral RNA silencing suppressors (VSRs) [86].
A hallmark of VSRs is their diversity: they can possess different amino acid sequences and target various stages of the RNA interference pathway. This diversity results in a wide spectrum of mechanisms for suppressing plant defense responses. The variation among VSRs enables viruses to effectively adapt to the defense systems of different host plant species [8].
The incorporation of VSR genes into viral vectors can enhance VIGS efficiency by improving the spread and accumulation of viral vectors within the plant. Some viral suppressors directly interfere with the silencing machinery in host plants. A well-characterized example is the 2b protein of Cucumber mosaic virus (CMV), belonging to the Bromoviridae family [40,62]. The 2b protein exhibits double-stranded RNA (dsRNA) binding activity, which is crucial for its pathogenicity. Expressed from a subgenomic RNA, it performs multiple functions: it determines symptoms associated with viral virulence, facilitates host-specific viral accumulation, inhibits RNA silencing, and supports the systemic spread of gene suppression [62,63,87,88].
The protein actively participates in regulating plant defense systems by disrupting the function of the RISC complex and proteins of the AGO family [63]. Another research application involves studying its effects on hormonal signaling pathways. It has been demonstrated that the 2b protein induces the accumulation of salicylic and jasmonic acids in infected plants while simultaneously suppressing the development of systemic acquired resistance through both pathways [87,88].
Some viral suppressors, such as the P19 protein of Tomato bushy stunt virus (TBSV, a member of the Tombusviridae family), bind to siRNAs, thereby blocking the formation of the active RISC complex [40,63]. The silencing suppressor B2 from Flock House virus (FHV) employs two distinct mechanisms of action: it can bind siRNAs and inhibit RNA interference similarly to the P19 suppressor. In VIGS experiments, FHV B2 has been utilized as a heterologous VSR that enhanced silencing efficiency when used with a BBWV2-based vector, particularly since it did not exacerbate BBWV2-induced symptoms in pepper [45,51].
The impact of viral suppressors on VIGS efficiency was convincingly demonstrated in a study by Zhou et al. [55]. This work employed the pTRV2-GFP-CaPDS vector, constructed based on the pTRV2-LIC vector. The modified vector was engineered with various VSRs: p19, HC-Pro, γb, 2b, and βb. Depending on the VSR used, the efficiency of PDS silencing in Capsicum annuum L. ranged from 3% to 93%. The highest silencing efficiency was observed in plants infected with the construct containing the 2b protein, while the lowest efficiency was seen with the βb protein. The combination of different VSRs also enhanced efficiency in the described experiment.
In conclusion, VSRs are powerful viral proteins that can enhance the spread and accumulation of viral vectors within plants, thereby increasing gene silencing efficiency. However, their inherent function is to antagonize the plant’s RNAi machinery, and their effects can be highly specific. Therefore, their application in VIGS requires careful optimization to balance silencing enhancement with potential unintended effects on plant physiology and result interpretation.

3.2. Choosing an Insert

The length of the insert is a primary determinant of success. Excessively short inserts often fail to induce effective silencing. This was systematically investigated by Liu and Page 2008 [74], who cloned fragments of the PDS gene ranging from 54 to 2046 bp into a TRV vector. Their results showed that fragments between 192 and 1304 bp caused a significant reduction in PDS expression, whereas the 54 bp fragment was completely ineffective. Conversely, very long inserts can impede viral spread and reduce silencing efficiency. In a study targeting the PDS gene in cotton (Gossypium hirsutum) using a CLCrV vector, Gu et al., 2014 [47] tested inserts from 50 to 1000 bp. They found the most potent silencing with a 500 bp fragment. Notably, vectors carrying longer inserts of 800 or 1000 bp showed PDS expression levels comparable to the negative control, indicating a failure of the VIGS process. Furthermore, long inserts are prone to genetic instability and can be partially or completely deleted from the viral genome during replication. Rong Wang et al., 2016 [73] observed this phenomenon using a CMV vector with inserts of 100–600 bp; inserts longer than 400 bp were frequently lost in systemic tissues.
Beyond length, the nucleotide composition of the insert is also important. Liu and Page 2008 [74] also demonstrated that the addition of 24-nucleotide homopolymer sequences (poly-A or poly-G tracts) to the ends of the PDS insert significantly attenuated the silencing effect in the TRV system, highlighting the need for careful sequence design.
A recent study demonstrated an innovative approach to optimizing insert length [89]. The authors showed that the insert length could be reduced by 10-fold to 24–32 bp. Remarkably, this not only maintained gene suppression efficiency but also enabled more accurate transcript quantification in RNA-seq analysis by eliminating artifacts. Additionally, the authors highlighted the importance of considering functional gene redundancy when selecting target sequences.
Thus, to ensure effective silencing, it is recommended to use two types of inserts: traditional 200–300 bp fragments or innovative ultra-short ones. A critical aspect of their design is accounting for orthologous genes to overcome functional redundancy.

3.3. Methods of Delivery of Agrobacteria

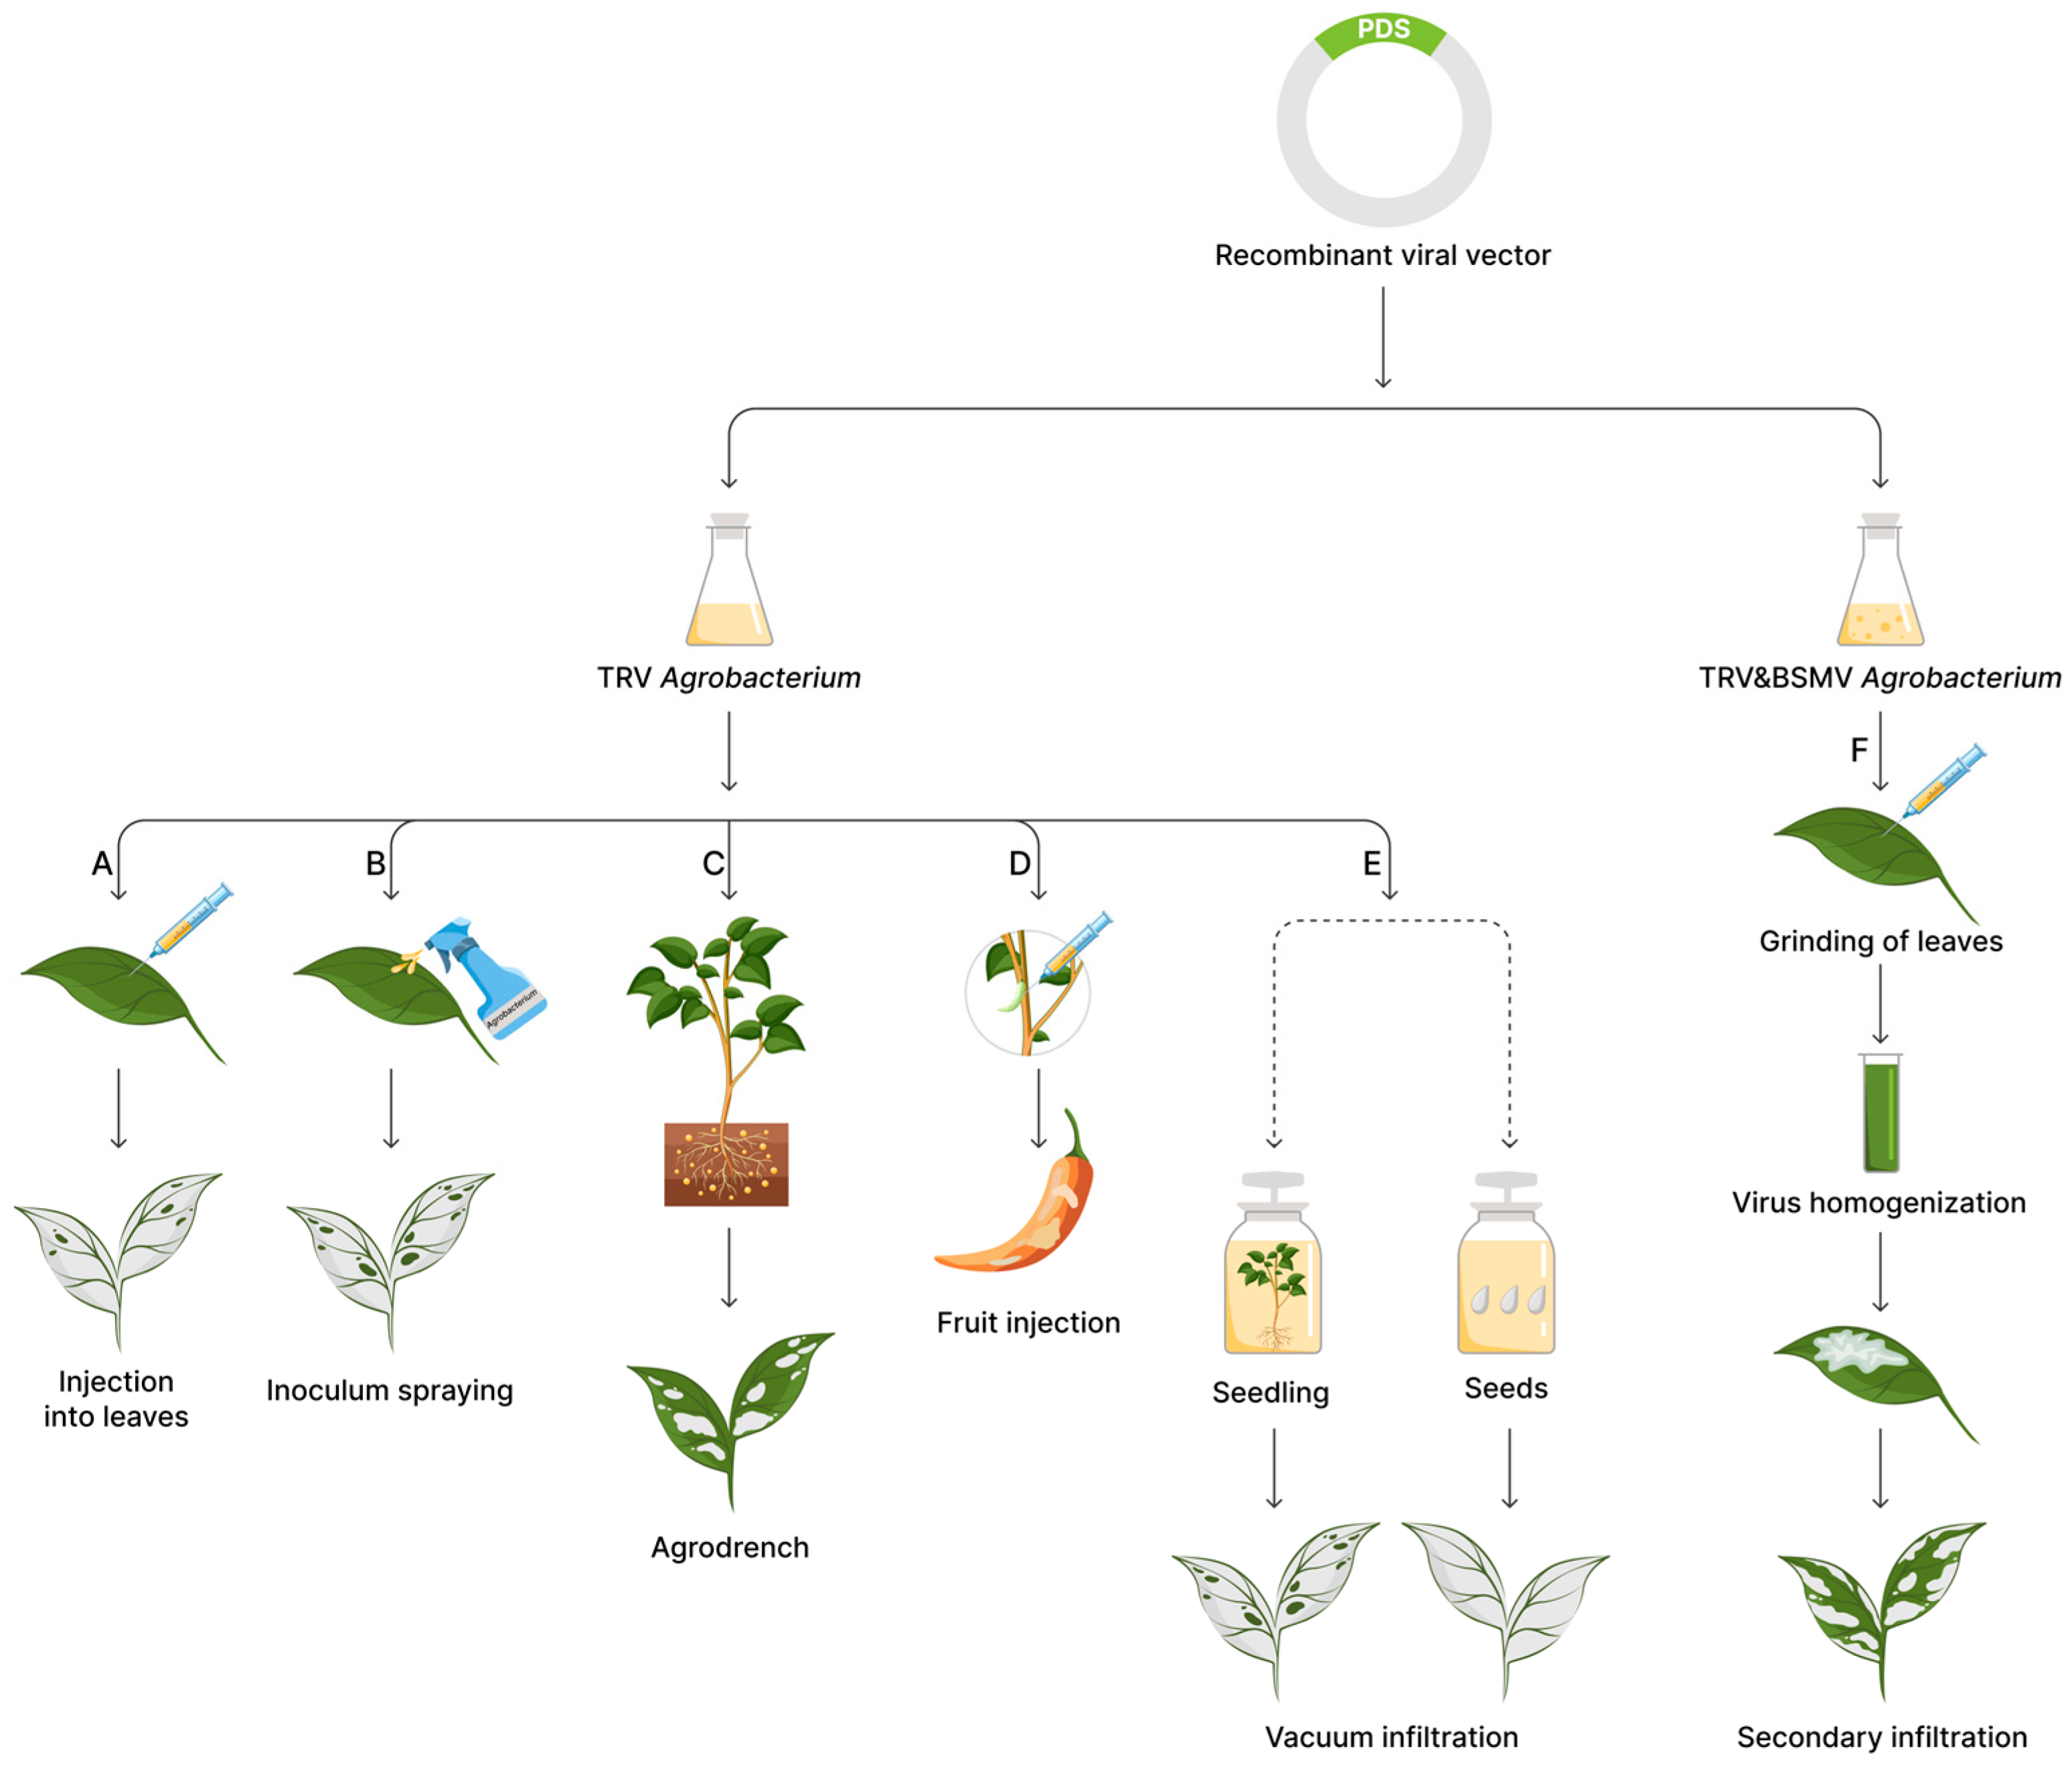
Viral vectors are delivered using Agrobacterium tumefaciens. The various delivery methods, each with distinct advantages and limitations, are summarized in Figure 7.
An important part in the study of genes is the choice of the method of delivery of agrobacteria carrying the viral vector into the plant. The choice of a specific delivery method depends on the type of plant, its morphological features, and research objectives. The effectiveness of virus-induced gene silencing (VIGS) can vary significantly depending on the chosen method of infection and the plant being infected. For example, for sunflower Helianthus annuus [76], the best method of infection is seed treatment under vacuum infiltration conditions. For the infection of monocotyledonous plants, there is information about the use of the secondary infiltration method [73,77].
For plants of the Solanaceae family, the infiltration of leaves by agrobacteria is considered the best method of delivering viral vectors. In a study by Meng et al. [78] three methods of infiltration of S. rostratum were used: leaf infiltration, cotyledon infiltration, and vacuum infiltration of sprouts. Among the infiltration methods used, infiltration of leaves or cotyledons with silencing efficiency of 100% and 88%, respectively, was found to be much more effective. The high efficiency of the agrodrench method was demonstrated on N. benthamiana in the work of Ryu et al. [79]. Furthermore, combining the agrodrench method with leaf infiltration significantly enhances gene silencing efficiency.
Leaf infiltration is most often used in VIGS experiments with Capsicum annuum L. and other pepper species [32,33,34,90,91,92,93,94,95,96,97,98,99]. However, there is an example of work in which the methods of agrodrench [100] and vacuum infiltration [99] were used for infection. The method of agroinjection of fruits was also used to study the genes regulating fruit color [101].
The analysis confirms the absence of a universal Agrobacterium delivery method for VIGS. The selection of an optimal protocol is critically determined by the biological characteristics of the target crop, specifically its species, morphology, and ontogenetic stage. As research shows, for plants of the Solanaceae family, such as pepper (Capsicum annuum L.), the most effective and widespread technique is the infiltration of leaves or cotyledons. In contrast, for other species, such as cereals or sunflower, vacuum infiltration of seedlings or seed treatment is preferable.
A key principle is matching the delivery method to the tissue localization of the gene under study. For analyzing the functions of genes active in roots, leaf infiltration is not suitable. Instead, methods such as vacuum infiltration of seedlings, agrodrench (flooding the soil with the suspension), or direct root soaking should be employed. However, the latter methods require careful optimization, as they can cause stress and tissue damage, potentially distorting the phenotype and experimental results.
Thus, the success of a VIGS experiment is determined not only by the vector design but also by the informed choice of an inoculation method tailored to the specific research question and the biology of the target organism.

3.4. The Growth Stage

The developmental stage of the host plant at the time of inoculation is a decisive factor for the success of VIGS, and although early stages hold an advantage, the optimal infection period depends on the plant family and species. For example, the work of Kim et al. by optimizing VIGS for soybeans, Glycine max confirmed that suppressing plant genes with the first opening leaf is much more effective than in plants at another stage of development [17]. In the work of Hartl et al. by optimizing VIGS for S.nigrum results were obtained according to which plants infected at the stage of 3–4 true leaves showed a low efficiency of PDS gene silencing compared with infected one-week-old seedlings [75].
For Capsicum annuum L. the optimal infection period is at the 2–4 true leaf stage. This was demonstrated in the work of Wang et al. [35], who investigated the effect of infection timing on silencing efficacy in pepper. Plants inoculated at the 2–4 true leaf stage showed a 90–100% rate of PDS gene silencing. In contrast, silencing was significantly less effective and its onset delayed in older plants at the 6–8 true leaf stage.
The growth stage of the plant at inoculation is a critical determinant of VIGS efficiency. The presented data consistently demonstrate that the juvenile phase of development provides the highest silencing efficacy across diverse plant species. An important exception applies when targeting genes expressed in reproductive organs or fruits, requiring later inoculation to ensure the silencing signal reaches the relevant tissues. Thus, the optimal timing is a compromise between peak systemic efficiency and the specific biological process under investigation.

3.5. Agroinoculate Concentration

The concentration of the agroinoculate (a mixture of agrobacteria) used to infect plants affects the final result of the experiment. Like the stage of growth, the optimal concentrations of the agroinoculate for infection depend on the plant species. According to the work of He et al. [80] the optimal concentration of agrobacteria for Miscanthus sinensis is OD600 = 0.7. At lower or higher concentrations of agrobacteria, the efficiency of gene silencing decreased significantly. In Glycine max, on the contrary, different concentrations of the agroinoculate had little effect on the effectiveness of gene silencing. However, plants infected with agrobacteria at the concentration of OD600 = 1.0–2.0 demonstrated the most effective gene silencing [17].
In a study by Wang et al. [35] above Capsicum annuum L., it was also noted that the concentration of OD600 = 0.8–1.0 causes a gene knockdown in greater cases than at lower concentrations of the agroinoculum. The silencing efficiency of plant genes infected with concentrations of OD600 = 2.0 and OD600 = 3.0 agrobacteria was not only noticeably lower, but more plants died at such high concentrations of the injected agroinoculum. Thus, the concentration of agrobacteria is a significant factor in infection.
The presented analysis demonstrates that there is no universal optimal concentration of agrobacteria for VIGS, and this parameter requires individual optimization for each plant species. However, it is important to note that the available data largely overlook the contribution of intra-specific genetic diversity. It is highly likely that the optimal concentration ranges may vary for different genotypes within a single species, which opens a direction for future more detailed investigations.

3.6. Plant Genotype

In the VIGS experiments, the effectiveness of silencing genotypes (varieties) of the same plant species differed significantly from each other. For example, in the work of Mardini et al. the silencing of genes with several sunflower genotypes was evaluated, and each sunflower variety has different silencing values: from 62% to 91% [76]. In an article by Wang et al. a PDS gene silencing experiment was conducted using three pepper varieties (Capsicum annuum L.). The results of the gene knockdown by variety: 64%, 77%, 94%. Based on the results obtained, the Early Calwonder variety with the most numerous cases of gene silencing was selected for further experiment [35].
Another example of varietal specificity is given by Kim et al., where VIGS optimization was performed using several varieties of Glycine max soybeans [17]. Jangyeobkong soybeans showed the most pronounced symptoms of PDS silencing: the silencing efficiency of the gene was 73%, therefore, this variety was used in the study of other parameters affecting the success of VIGS. The effectiveness of PDS suppression in the other two Glycine max genotypes was 60% or less.
These findings highlight a fundamental principle: the success of VIGS is not uniform across a species but is strongly influenced by the plant’s genetic background. The consistent observation of a wide range of silencing efficiencies (e.g., 62–94% in pepper, 60–73% in soybean) among different genotypes necessitates the preliminary identification of highly amenable varieties for reliable results. This genotypic dependency must be considered a key variable alongside other optimization parameters.

3.7. Environmental Factors: Temperature, Humidity, Photoperiod

The external conditions in which infected plants grow are of great importance. Environmental factors such as temperature [35,80,81,82,83], photoperiod [17,84], and humidity [81] affect the reproduction and spread of the viral vector throughout the plant, which affects the effectiveness of gene silencing.
Plant growth temperature is the first determining factor in the development of gene silencing in plants. The optimal temperature for conducting VIGS depends on the type of plant. For example, in the experiment of Wang et al. according to VIGS Capsicum annuum L. optimization, infected plants were grown at temperatures of 18–28 °C. Plants that were grown at temperatures of 20–25 °C demonstrated high VIGS efficiency compared to temperatures of 18 °C and 28 °C, respectively [35]. In an experiment on the effect of temperature on VIGS (for instance, N. benthamiana), infected plants growing at low temperatures showed more severe symptoms of infection with the viral vector [81]. Too low a temperature reduces the activity of RNA interference proteins, which contributes to an increase in the number of viral vectors in the plant and its spread [82]. At high temperatures, there is a decrease in the concentration of viral vectors, which also impairs the effectiveness of silencing [83].
The percentage of humidity at which plants grow can affect the time after which the symptoms of gene silencing appear. In the study by Fu et al. it was found that at 30% humidity, depigmentation of S. lycopersicum leaves due to PDS gene silencing was manifested 1–3 weeks later than at 60% humidity. At low temperature and humidity, the first manifestation of PDS silencing symptoms was recorded 8 weeks after infection, but silencing activity was present for up to 4 months [81].
There is a remarkable gap in the literature regarding the role of photoperiod in enhancing VIGS efficiency in Solanaceae plants. However, in a paper on VIGS optimization for Glycine max, Kim et al. the effect of photoperiod on VIGS efficiency was investigated. The results of the experiment with different lighting periods showed that Glycine max grown under photoperiod 16/8 (16 h under light, 8 h under darkness) showed symptoms of PDS silencing in 100% of cases, while samples grown under photoperiods 12/12 and 8/16 showed symptoms of PDS silencing only in 70% and 20% of cases, respectively [17].
In the work on VIGS optimization in A. thaliana, a significant influence of the photoperiod on the experimental results was also noted. In the experiment, one group of TRV-PDS inoculated plants was cultivated under photoperiod 16/8, the other group was cultivated under photoperiod 8/16. Symptoms of PDS silencing were observed in 90–100% of cases in the first group, and only 10% of cases were observed in the second group [84].
To increase the effectiveness of silencing, infected plants can be placed in a dark, cool (~17 °C) place for 2 days [76,81]. The introduction of this stage improves the replication of the viral vector, and promotes the spread of the virus through the plant.
According to the results of the above studies, the effectiveness of VIGS is always determined by numerous factors, from the choice of gene insertion into the viral vector and the method of infection to the concentration of agroinoculate and plant growth factors.
Environmental conditions—temperature, humidity, and photoperiod—collectively operate as an integrated control system for VIGS efficiency. Temperature dictates the balance between RNAi machinery activity and viral accumulation, humidity modulates the speed of systemic signaling, and photoperiod provides the energy and regulatory cues necessary for robust silencing. The absence of a universal optimum for these parameters highlights a critical layer of species-specific protocol optimization.

4. Application of VIGS for Functional Genomics of Plants

Capsicum annuum L. is a globally significant vegetable crop with substantial economic and nutritional value. However, functional genomic studies in pepper have been challenging due to its large genome and limited sequence information. Virus-induced gene silencing (VIGS) has emerged as a powerful reverse genetics tool to overcome these limitations, enabling rapid functional characterization of genes. This section reviews the application of VIGS in elucidating gene functions related to key agronomic traits in pepper, including fruit quality, plant architecture, and stress resilience.

4.1. Fruit Quality and Pigmentation

VIGS has been extensively employed to dissect the genetic pathways controlling fruit color and biochemical composition, which are critical for consumer preference and breeding.
Anthocyanin biosynthesis. The R2R3 MYB transcription factor encoded by CaAN2 is a master regulator of anthocyanin biosynthesis. VIGS-mediated silencing of CaAN2 abolished purple pigmentation in leaves, flowers, and fruits [91]. In genotypes where CaAN2 is not expressed, a fruit-specific locus, CaAN3, was identified, and its role as an activator of anthocyanin biosynthesis was confirmed via VIGS [92]. Furthermore, UV-induced anthocyanin accumulation in fruits was shown to involve CaWRKY transcription factors that bind to promoters of structural genes in this pathway [34]. These pigments may also contribute to defense against phytopathogens [90].
Carotenoid biosynthesis and fruit color. The vibrant colors of ripe pepper fruits are determined by the degradation of chlorophyll and the accumulation of carotenoids. Virus-induced gene silencing (VIGS) of the CaRIN transcription factor, a key regulator of ripening, demonstrated its critical role by resulting in increased chlorophyll content, reduced carotenoid accumulation, and uneven fruit coloration [102]. Furthermore, targeted suppression of its direct downstream target, CaLhcb-P4, via VIGS accelerated chlorophyll degradation, confirming its functional role in this regulatory pathway. Complementing these findings on chlorophyll metabolism, VIGS-based silencing of key carotenogenic genes, including phytoene synthase (Psy), capsanthin/capsorubin synthase (Ccs), lycopene-β-cyclase (Lcyb), and β-carotene hydroxylase (Crtz), resulted in altered fruit coloration, such as shifts to orange or yellow [32]. Specifically, suppression of CaPSY1 led to increased lutein and decreased zeaxanthin content [101]. Silencing of the PRR2 gene resulted in white pigmentation in both immature and mature fruits [33].
Pungency (capsaicinoid biosynthesis). Pungency is a hallmark trait of chili peppers. VIGS studies, coupled with High-Performance Liquid Chromatography (HPLC), have highlighted the essential role of the Pun1-encoded capsaicin synthase in capsaicinoid biosynthesis. The enzyme pAMT (vanillylamine synthase), responsible for converting vanillin to vanillylamine, was also characterized, revealing high vanillylamine content in sweet pepper varieties [34]. Research on genes modulating pungency is vital for breeding peppers with desired flavor profiles.

4.2. Plant Architecture and Developmental Processes

While less explored, VIGS has provided insights into genes governing plant growth, development, and morphology.
Reproductive development and fertility. A landmark study combined Bulked segregant analysis (BSA-Seq) with VIGS to identify and validate the msc-2 gene, a key regulator of male sterility in pepper. The candidate gene, Capana05g000766, harbors a “T” deletion leading to the loss of its PHD domain. VIGS-mediated knockdown of this gene successfully induced male sterility, confirming its critical role in tapetum development and pollen fertility. This work not only explains a component of the genetic network controlling pollen formation but also provides a valuable molecular marker for marker-assisted breeding programs [103].
General growth and development. Proteins SGT1 and Skp1 are integral to ubiquitin ligase complexes. Their silencing via VIGS induced dwarfism and plant mortality. Notably, these symptoms were absent under sterile conditions, indicating that CaSgt1 and CaSkp1 are essential for fundamental growth processes and development, in addition to pathogen defense [99].
Leaf and flower development. The role of anthocyanins in leaves was demonstrated by silencing the CaMYB gene, which affected leaf pigmentation and potentially defense mechanisms [90]. Although direct studies on flower development are limited, VIGS has been applied to genes like An2, which affects floral pigmentation [91], confirming the method’s applicability for studying reproductive tissues.

4.3. Resistance to Biotic Stresses

VIGS is a key technique for identifying genes involved in pepper’s defense responses against pathogens and pests.
Bacterial and oomycete resistance. The transcription factor CaPHL8 was identified as a positive regulator of immunity against Ralstonia solanacearum [98]. Similarly, CaWRKY40 and CaWRKY58 contribute to resistance against this bacterium [96]. Defense against the oomycete Phytophthora capsici involves peroxidases CaPOD [95], the CaRGA2 gene [97], and CaPTI1, whose suppression compromised defense signaling [100].
Insect resistance. The jasmonate pathway gene CaLOX2 is crucial for induced defense against Western flower thrips. Silencing CaLOX2 reduced jasmonic acid levels and increased plant susceptibility to this pest [93].

4.4. Tolerance to Abiotic Stresses

VIGS has elucidated molecular mechanisms behind pepper’s adaptation to environmental challenges.
Temperature stress. Thermotolerance is regulated by CaWRKY45 [96], while cold tolerance is mediated by F-box family genes LTSF1 and LTSF2 [104].
Salt and osmotic stress. The transcription factor CaMADS and the CaPTI1 gene play pivotal roles in the response to cold, salt, and osmotic stress in pepper [94,100]. Further expanding the understanding of stress response mechanisms, functional analysis using VIGS revealed that the CaTPS1 gene, encoding a key enzyme in trehalose biosynthesis, is also critical for salt and cold tolerance [105]. Suppression of CaTPS1 expression significantly impaired the plant’s stress response, leading to reduced chlorophyll content and decreased activity of key antioxidant enzymes, which underscores its essential role in pepper’s adaptation to abiotic stress.
In conclusion, the extensive application of VIGS has been instrumental in advancing the functional genomics of Capsicum annuum L. To date, research has predominantly illuminated the genetic basis of economically critical traits like fruit quality and stress resistance. Moving forward, a major opportunity lies in expanding the application of VIGS to unravel the genetic networks governing plant architecture, leaf development, and floral organogenesis, areas that remain less charted.

5. Advantages, Limitations, and Future Perspectives of VIGS in Pepper Genomics

VIGS has emerged as a pivotal tool for functional genomics in pepper, yet its application is accompanied by specific limitations and vast potential for future development.

5.1. Limitations and Practical Challenges

The implementation of VIGS faces several practical constraints. A significant limitation is its reliance on genetically modified viral vectors, which often necessitates conducting experiments under strict containment conditions. Furthermore, the viral infection itself can cause physiological stress and unintended phenotypic effects, potentially confounding the interpretation of silencing results. The efficiency of VIGS is also highly dependent on the plant genotype, which can influence viral replication and systemic spread [35]. Finally, the technique is less suitable for studying traits that manifest late in reproduction or require long-term, stable gene silencing.

5.2. Key Advantages over Stable Transformation

Despite these challenges, VIGS offers distinct advantages over traditional methods for gene suppression, such as generating stable transgenic plants with inverted repeat constructs [35].
Speed and simplicity. The procedure is relatively fast. Functional gene silencing can be achieved within weeks, bypassing the lengthy process of stable transformation and regeneration. Furthermore, VIGS vector construction is more straightforward than generating constructs for stable transformation. It typically involves cloning a single, short sense fragment of the target gene into a plasmid carrying the viral genome. This avoids the technical challenges of assembling complex inverted repeat constructs, which are often unstable and can undergo recombination during propagation in bacterial hosts.
Transient and controllable silencing. A key advantage is the transient nature of VIGS. This allows for the spatial and temporal analysis of gene function, which is crucial for studying genes essential for plant viability. While stable knockout mutants of such genes are often lethal, VIGS produces a partial, non-uniform silencing that enables the plant to survive, permitting functional analysis in developing tissues.
High-throughput and multiplexing potential. The speed of VIGS makes it ideal for high-throughput functional screening of numerous candidate genes. Additionally, the technology allows for the simultaneous silencing of multiple genes, either through the use of a single vector containing tandem target sequences or by exploiting sequence homology between related genes [106].

5.3. Future Perspectives: Integrating VIGS with Multi-Omics Technologies

To further enhance the utility of VIGS in pepper functional genomics, future research could strategically focus on its integration with other advanced technologies. Such a synergistic approach would provide a more comprehensive understanding of gene function and regulatory networks.
One promising strategy involves coupling VIGS with subsequent transcriptomic (e.g., RNA-Seq) and metabolomic analyses. For instance, following the silencing of a transcription factor suspected to regulate fruit shape or capsaicinoid biosynthesis, RNA-Seq could be employed. This would not only confirm the successful downregulation of the target gene but, more importantly, could reveal the entire cascade of downstream transcriptional changes. Such an analysis can identify differentially expressed genes across critical pathways—including metabolism, hormone signaling, and cellular communication—thereby allowing researchers to reconstruct the regulatory network controlled by the transcription factor. Concurrent metabolomic profiling would be highly advisable to quantify the resulting biochemical changes, such as alterations in capsaicinoid levels or cell wall composition, thereby directly linking the transcriptional rewiring to the ultimate phenotypic outcome [32,34,90,101].
Proposed research directions for key traits: This integrated VIGS-omics pipeline could be valuably applied to resolve several pressing questions in pepper biology:
Fruit shape and architecture: Key regulators of ovary development and fruit morphology might be identified by silencing candidate genes from QTL mapping studies and analyzing subsequent changes in the transcriptome and hormone profiles.
Plant architecture: Investigating genes controlling branching, plant height, and leaf development could be achieved through VIGS of homologs of known genes from other species, followed by detailed phenotyping and transcriptomics to uncover the genetic basis of pepper’s unique growth habit.
Pericarp color and composition: Research could expand beyond the well-studied anthocyanin and carotenoid pathways to discover novel regulators of chlorophyll degradation and wax biosynthesis, which are significant contributors to final fruit color and gloss.
Capsaicinoid regulation: A systematic approach to silencing candidate genes from biosynthetic and putative regulatory clusters, combined with metabolomics, would enable a more precise mapping of the capsaicinoid pathway and help identify its key control points.

6. Conclusions

Virus-induced gene silencing has established itself as a key technology in plant functional genomics, particularly for complex species such as Capsicum annuum L. This comprehensive review systematically analyzed the main factors determining the efficiency of VIGS in pepper, emphasizing the complex interplay between vector selection, insert design, inoculation methodology, and environmental conditions that collectively determine experimental success. The optimization of these parameters, such as the use of TRV-based vectors, agroinfiltration at the 2–4 true leaf stage, control of temperature and photoperiod, and the application of viral suppressors of RNA silencing, has been critical for establishing reliable and reproducible protocols in this recalcitrant species.
The application of optimized VIGS protocols has led to significant advancements in deciphering the genetic basis of key agronomic traits in pepper. In the area of fruit quality, the technology has enabled the functional characterization of genes controlling anthocyanin (CaAN2, CaAN3, CaMYB), carotenoid (CaPSY1, Ccs, Lcyb, Crtz, PRR2, CaRIN, CaLhcb-P4), and capsaicinoid (Pun1, pAMT) biosynthesis. In the sphere of stress resistance, VIGS has been instrumental in identifying components of the immune response (CaWRKY40, CaWRKY58, CaPHL8, CaRGA2, CaPTI1, CaPOD) and genes conferring tolerance to abiotic factors (CaWRKY45, LTSF1/LTSF2, CaPTI1, CaTPS1, CaMADS), as well as the role of CaLOX2 in defense against insect pests. Regarding plant architecture and developmental processes, VIGS has confirmed the function of the msc-2 gene in controlling male sterility and characterized CaSgt1 and CaSkp1 as essential for fundamental growth processes.
Looking forward, the integration of VIGS with multi-omics approaches represents the most promising direction for future research. Combining targeted gene silencing with transcriptomic and metabolomic analyses will help unravel complex regulatory networks and the polyfunctionality of identified genes. Priority should be given to the systematic study of pleiotropic effects of key regulators of growth, development, and stress tolerance, particularly in the context of pepper’s unique metabolic pathways and stress adaptation mechanisms.
Although VIGS has certain limitations related to its transient nature and the need for species-specific optimization, its unique advantages, such as speed, cost-effectiveness, and applicability to genetically challenging species like pepper, ensure its continued importance in plant functional genomics. As genomic resources for Capsicum annuum L. continue to expand through advanced sequencing technologies, VIGS will remain an essential methodology for bridging the gap between genetic sequence and biological function, ultimately contributing to the development of improved, resilient pepper varieties.

Author Contributions

Conceptualization, M.D.; validation, A.S., K.D. and M.D.; resources, M.D.; data curation, A.R. and M.G.; writing—original draft preparation, A.S., A.R. and M.G.; writing—review and editing, A.S., A.R., M.G., K.D. and M.D.; visualization, A.R. and M.G.; supervision, M.D.; project administration, M.D. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Data Availability Statement

No new data were created or analysed in this study.

Conflicts of Interest

The authors declare no conflicts of interest.

Abbreviations

The following abbreviations are used in this manuscript:
VIGSVirus-induced gene silencing
PTGSPost-transcriptional gene silencing
PDSPhytoene desaturase
siRNASmall interference RNA
miRNAMicroRNA
dsRNADouble stranded RNA
TRVTobacco rattle virus

References

  1. Xie, L.; Gong, X.; Yang, K.; Huang, Y.; Zhang, S.; Shen, L.; Sun, Y.; Wu, D.; Ye, C.; Zhu, Q.-H.; et al. Technology-enabled great leap in deciphering plant genomes. Nat. Plants 2024, 10, 551–566. [Google Scholar] [CrossRef] [Scilit]
  2. Zhang, D.; Zhang, Z.; Unver, T.; Zhang, B. CRISPR/Cas: A powerful tool for gene function study and crop improvement. J. Adv. Res. 2020, 29, 207–221. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Liu, Q.; Lin, L.; He, S.; Yu, J.; Xie, C.; Gai, C.; Han, Y.; Liu, C.; Huang, F.; Chen, D.; et al. A simple and efficient TALEN system for genome editing in plants. Plant Mol. Biol. 2025, 115, 25. [Google Scholar] [CrossRef] [Scilit]
  4. Bhuyan, S.J.; Kumar, M.; Devde, P.R.; Rai, A.C.; Mishra, A.K.; Singh, P.K.; Siddique, K.H.M. Progress in gene editing tools, implications and success in plants: A review. Front. Genome Ed. 2023, 5, 1272678. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  5. Ma, L.; Kong, F.; Sun, K.; Wang, T.; Guo, T. From Classical radiation to modern radiation: Past, present, and future of radiation mutation breeding. Front. Public Health 2021, 9, 768071. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Chen, L.; Duan, L.; Sun, M.; Yang, Z.; Li, H.; Hu, K.; Yang, H.; Liu, L. Current trends and insights on EMS mutagenesis application to studies on plant abiotic stress tolerance and development. Front. Plant Sci. 2023, 13, 1052569. [Google Scholar] [CrossRef] [Scilit]
  7. Ram, H.; Soni, P.; Salvi, P.; Gandass, N.; Sharma, A.; Kaur, A.; Sharma, T.R. Insertional mutagenesis approaches and their use in rice for functional genomics. Plants 2019, 8, 310. [Google Scholar] [CrossRef] [Scilit]
  8. Zulfiqar, S.; Farooq, M.A.; Zhao, T.; Wang, P.; Tabusam, J.; Wang, Y.; Xuan, S.; Zhao, J.; Chen, X.; Shen, S.; et al. Virus-Induced Gene Silencing (VIGS): A Powerful Tool for Crop Improvement and Its Advancement towards Epigenetics. Int. J. Mol. Sci. 2023, 24, 5608. [Google Scholar] [CrossRef] [Scilit]
  9. Liu, Y.; Lyu, R.; Singleton, J.J.; Patra, B.; Pattanaik, S.; Yuan, L. A Cotyledon-based Virus-Induced Gene Silencing (Cotyledon-VIGS) approach to study specialized metabolism in medicinal plants. Plant Methods 2024, 20, 26. [Google Scholar] [CrossRef] [Scilit]
  10. Kumagai, M.H.; Donson, J.; Della-Cioppa, G.; Harvey, D.; Hanley, K.; Grill, L.K. Cytoplasmic inhibition of carotenoid biosynthesis with virus-derived RNA. Proc. Natl. Acad. Sci. USA 1995, 92, 1679–1683. [Google Scholar] [CrossRef] [Scilit]
  11. Rössner, C.; Lotz, D.; Becker, A. VIGS goes Viral: How VIGS transforms our understanding of plant science. Annu. Rev. Plant Biol. 2022, 73, 703–728. [Google Scholar] [CrossRef] [Scilit]
  12. Cui, H.; Wang, A. An efficient viral vector for functional genomic studies of Prunus fruit trees and its induced resistance to Plum pox virus via silencing of a host factor gene. Plant Biotechnol. J. 2016, 15, 344–356. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  13. Villar-Álvarez, D.; Navarro, J.A.; Pallas, V.; Sanchez-Navarro, J.Á. Engineering VIGS vectors by modifying movement proteins of the 30K family. Biotechnol. J. 2024, 19, e202400584. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  14. Tian, Y.; Fang, Y.; Zhang, K.; Zhai, Z.; Yang, Y.; He, M.; Cao, X. Applications of Virus-Induced Gene silencing in cotton. Plants 2024, 13, 272. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Liu, Y.; Schiff, M.; Dinesh-Kumar, S.P. Virus-induced gene silencing in tomato. Plant J. 2002, 31, 777–786. [Google Scholar] [CrossRef] [Scilit]
  16. Holzberg, S.; Brosio, P.; Gross, C.; Pogue, G.P. Barley stripe mosaic virus-induced gene silencing in a monocot plant. Plant J. 2002, 30, 315–327. [Google Scholar] [CrossRef] [Scilit]
  17. Kim, K.H.; Lim, S.; Kang, Y.J.; Yoon, M.Y.; Nam, M.; Jun, T.H.; Seo, M.-J.; Baek, S.-B.; Lee, J.-H.; Moon, J.-K.; et al. Optimization of a Virus-Induced Gene Silencing System with Soybean yellow common mosaic virus for Gene Function Studies in Soybeans. Plant Pathol. J. 2016, 32, 112–122. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Mustafa, R.; Shafiq, M.; Mansoor, S.; Briddon, R.W.; Scheffler, B.E.; Scheffler, J.; Amin, I. Virus-Induced Gene Silencing in Cultivated Cotton (Gossypium spp.) Using Tobacco Rattle Virus. Mol. Biotechnol. 2015, 58, 65–72. [Google Scholar] [CrossRef] [Scilit]
  19. Robertson, D. VIGS vectors for gene silencing: Many targets, many tools. Annu. Rev. Plant Biol. 2004, 55, 495–519. [Google Scholar] [CrossRef] [Scilit]
  20. Hayward, A.; Padmanabhan, M.; Dinesh-Kumar, S.P. Virus-Induced Gene Silencing in Nicotiana benthamiana and Other Plant Species. In Plant Reverse Genetics: Methods and Protocols; Methods in Molecular Biology; Humana Press: Totowa, NJ, USA, 2010; pp. 55–63. [Google Scholar] [CrossRef] [Scilit]
  21. Shi, G.; Hao, M.; Tian, B.; Cao, G.; Wei, F.; Xie, Z. A methodological advance of tobacco rattle Virus-Induced gene silencing for functional genomics in plants. Front. Plant Sci. 2021, 12, 671091. [Google Scholar] [CrossRef] [Scilit]
  22. Zeng, H.; Xie, Y.; Liu, G.; Wei, Y.; Hu, W.; Shi, H. Agrobacterium-Mediated Gene Transient Overexpression and Tobacco Rattle Virus (TRV)-Based Gene silencing in Cassava. Int. J. Mol. Sci. 2019, 20, 3976. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  23. Wieczorek, P.; Obrępalska-Stęplowska, A. Suppress to Survive—Implication of plant viruses in PTGS. Plant Mol. Biol. Report. 2014, 33, 335–346. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  24. Manmathan, H.; Shaner, D.; Snelling, J.; Tisserat, N.; Lapitan, N. Virus-induced gene silencing of Arabidopsis thaliana gene homologues in wheat identifies genes conferring improved drought tolerance. J. Exp. Bot. 2013, 64, 1381–1392. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  25. Jupin, I. A protocol for VIGS in Arabidopsis thaliana using a One-Step TYMV-Derived vector. In Virus-Induced Gene Silencing: Methods and Protocols; Methods in Molecular Biology; Humana Press: Totowa, NJ, USA, 2013; pp. 197–210. [Google Scholar] [CrossRef] [Scilit]
  26. Li, Q.X.; Wang, J.; Zheng, S.; Yang, N.; Sun, K.; He, C.Y. Virus-induced gene silencing in Nicotiana benthamiana triggered by heterologous gene sequences from Viola philippica. Biol. Plant. 2018, 63, 153–163. [Google Scholar] [CrossRef] [Scilit]
  27. Senthil-Kumar, M.; Wang, M.; Chang, J.; Ramegowda, V.; Del Pozo, O.; Liu, Y.; Doraiswamy, V.; Lee, H.; Ryu, C.; Wang, K.; et al. Virus-induced gene silencing database for phenomics and functional genomics in Nicotiana benthamiana. Plant Direct 2018, 2, e00055. [Google Scholar] [CrossRef] [Scilit]
  28. Chen, Z.J.; Wang, J.; Tian, L.; Lee, H.-S.; Wang, J.J.; Chen, M.; Lee, J.J.; Josefsson, C.; Madlung, A.; Watson, B.; et al. The development of an Arabidopsis model system for genome-wide analysis of polyploidy effects. Biol. J. Linn. Soc. 2004, 82, 689–700. [Google Scholar] [CrossRef] [Scilit]
  29. Dzhos, E.A.; Shumilina, D.V.; Pyshnaya, O.N.; Mamedov, M.I.; Baikov, A.A.; Matyukina, A.A. Creation of an interspecific hybrid of Capsicum annuum L. and C. frutescens L. using biotechnological approaches. Veg. Crops Russ. 2021, 4, 27–33. [Google Scholar] [CrossRef] [Scilit]
  30. Zhuang, Y.; Chen, L.; Sun, L.; Cao, J. Bioactive characteristics and antioxidant activities of nine peppers. J. Funct. Foods 2012, 4, 331–338. [Google Scholar] [CrossRef] [Scilit]
  31. Wahba, N.M.; Ahmed, A.S.; Ebraheim, Z.Z. Antimicrobial effects of pepper, parsley, and dill and their roles in the microbiological quality enhancement of traditional Egyptian Kareish cheese. Foodborne Pathog. Dis. 2009, 7, 411–418. [Google Scholar] [CrossRef] [Scilit]
  32. Tian, S.-L.; Li, L.; Chai, W.-G.; Shah, S.N.M.; Gong, Z.-H. Effects of silencing key genes in the capsanthin biosynthetic pathway on fruit color of detached pepper fruits. BMC Plant Biol. 2014, 14, 314. [Google Scholar] [CrossRef] [Scilit]
  33. Jeong, H.-B.; Jang, S.-J.; Kang, M.-Y.; Kim, S.; Kwon, J.-K.; Kang, B.-C. Candidate Gene Analysis Reveals That the Fruit Color Locus C1 Corresponds to PRR2 in Pepper (Capsicum frutescens). Front. Plant Sci. 2020, 11, 399. [Google Scholar] [CrossRef] [Scilit]
  34. Wang, Y.; Liu, S.; Wang, H.; Zhang, Y.; Li, W.; Liu, J.; Cheng, Q.; Sun, L.; Shen, H. Identification of the regulatory genes of UV-B-Induced anthocyanin biosynthesis in pepper fruit. Int. J. Mol. Sci. 2022, 23, 1960. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Wang, J.E.; Li, D.W.; Gong, Z.H.; Zhang, Y.L. Optimization of virus-induced gene silencing in pepper (Capsicum annuum L.). Genet. Mol. Res. 2013, 12, 2492–2506. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Chung, E.; Seong, E.; Kim, Y.-C.; Chung, E.J.; Oh, S.-K.; Lee, S.; Park, J.M.; Joung, Y.H.; Choi, D. A Method of High Frequency Virus-induced Gene Silencing in Chili Pepper (Capsicum annuum L. cv. Bukang). Mol. Cells 2004, 17, 377–380. [Google Scholar] [CrossRef] [Scilit]
  37. Zaheer, U.; Munir, F.; Salum, Y.M.; He, W. Function and regulation of plant ARGONAUTE proteins in response to environmental challenges: A review. PeerJ 2024, 12, e17115. [Google Scholar] [CrossRef] [Scilit]
  38. Fang, X.; Qi, Y. RNAI in Plants: An Argonaute-Centered view. Plant Cell 2016, 28, 272–285. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Brosnan, C.A.; Voinnet, O. Cell-to-cell and long-distance siRNA movement in plants: Mechanisms and biological implications. Curr. Opin. Plant Biol. 2011, 14, 580–587. [Google Scholar] [CrossRef] [Scilit]
  40. Marttinen, E.M.; Lehtonen, M.T.; Van Gessel, N.; Reski, R.; Valkonen, J.P.T. Viral suppressor of RNA silencing in vascular plants also interferes with the development of the bryophyte Physcomitrella patens. Plant Cell Environ. 2021, 45, 220–235. [Google Scholar] [CrossRef] [Scilit]
  41. Csorba, T.; Kontra, L.; Burgyán, J. viral silencing suppressors: Tools forged to fine-tune host-pathogen coexistence. Virology 2015, 479–480, 85–103. [Google Scholar] [CrossRef] [Scilit]
  42. Pertermann, R.; Tamilarasan, S.; Gursinsky, T.; Gambino, G.; Schuck, J.; Weinholdt, C.; Lilie, H.; Grosse, I.; Golbik, R.P.; Pantaleo, V.; et al. A viral suppressor modulates the plant immune response early in infection by regulating MicroRNA activity. MBio 2018, 9, e00419-18. [Google Scholar] [CrossRef] [Scilit]
  43. Zhou, T.; Dong, L.; Jiang, T.; Fan, Z. Silencing specific genes in plants using Virus-Induced Gene Silencing (VIGS) vectors. In Plant Virology: Methods and Protocols; Methods in Molecular Biology; Springer: New York, NY, USA, 2021; pp. 149–161. [Google Scholar] [CrossRef] [Scilit]
  44. Unver, T.; Budak, H. Virus-Induced Gene Silencing, a post transcriptional gene silencing method. Int. J. Plant Genom. 2009, 2009, 198680. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Choi, B.; Kwon, S.-J.; Kim, M.-H.; Choe, S.; Kwak, H.-R.; Kim, M.-K.; Jung, C.; Seo, J.-K. A plant Virus-Based vector system for gene function studies in Pepper. Plant Physiol. 2019, 181, 867–880. [Google Scholar] [CrossRef] [Scilit]
  46. Otagaki, S.; Arai, M.; Takahashi, A.; Goto, K.; Hong, J.-S.; Masuta, C.; Kanazawa, A. Rapid induction of transcriptional and post-transcriptional gene silencing using a novel Cucumber mosaic virus vector. Plant Biotechnol. 2006, 23, 259–265. [Google Scholar] [CrossRef] [Scilit]
  47. Gu, Z.; Huang, C.; Li, F.; Zhou, X. A versatile system for functional analysis of genes and microRNAs in cotton. Plant Biotechnol. J. 2014, 12, 638–649. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  48. Zhu, X.H.; Dinesh-Kumar, S.P. Virus-induced gene silencing (VIGS) to study gene function in plants. In RNA Interference: Methods for Plants and Animals; CABI: Wallingford, UK, 2008; pp. 26–49. [Google Scholar] [CrossRef] [Scilit]
  49. Lange, M.; Yellina, A.L.; Orashakova, S.; Becker, A. Virus-Induced Gene Silencing (VIGS) in plants: An overview of target species and the Virus-Derived Vector Systems. In Virus-Induced Gene Silencing: Methods and Protocols; Methods in Molecular Biology; Humana Press: Totowa, NJ, USA, 2013; pp. 1–14. [Google Scholar] [CrossRef] [Scilit]
  50. Wang, Z.; Cao, S.; Xu, X.; He, Y.; Shou, W.; Munaiz, E.D.; Yu, C.; Shen, J. Application and expansion of Virus-Induced gene silencing for functional studies in vegetables. Horticulturae 2023, 9, 934. [Google Scholar] [CrossRef] [Scilit]
  51. Singh, G.; Popli, S.; Hari, Y.; Malhotra, P.; Mukherjee, S.; Bhatnagar, R.K. Suppression of RNA silencing by Flock house virus B2 protein is mediated through its interaction with the PAZ domain of Dicer. FASEB J. 2009, 23, 1845–1857. [Google Scholar] [CrossRef] [Scilit]
  52. Tang, Q.; Wei, S.; Chen, Z.; Zheng, X.; Tu, P.; Tao, F. The reverse genetic as a potential of virus-induced gene silencing in tomato biology. Food Front. 2024, 6, 2498–2514. [Google Scholar] [CrossRef] [Scilit]
  53. Martín-HernáNdez, A.M.; Baulcombe, D.C. Tobacco rattle virus 16-Kilodalton protein encodes a suppressor of RNA silencing that allows transient viral entry in meristems. J. Virol. 2008, 82, 4064–4071. [Google Scholar] [CrossRef] [Scilit]
  54. Zaidi, S.S.-E.-A.; Mansoor, S. Viral vectors for plant genome engineering. Front. Plant Sci. 2017, 8, 539. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  55. Zhou, Y.; Deng, Y.; Liu, D.; Wang, H.; Zhang, X.; Liu, T.; Wang, J.; Li, Y.; Ou, L.; Liu, F.; et al. Promoting virus-induced gene silencing of pepper genes by a heterologous viral silencing suppressor. Plant Biotechnol. J. 2021, 19, 2398–2400. [Google Scholar] [CrossRef] [Scilit]
  56. Tian, J.; Pei, H.; Zhang, S.; Chen, J.; Chen, W.; Yang, R.; Meng, Y.; You, J.; Gao, J.; Ma, N. TRV–GFP: A modified Tobacco rattle virus vector for efficient and visualizable analysis of gene function. J. Exp. Bot. 2013, 65, 311–322. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  57. Liu, H.; Fu, D.; Zhu, B.; Yan, H.; Shen, X.; Zuo, J.; Zhu, Y.; Luo, Y. Virus-induced Gene Silencing in Eggplant (Solanum melongena). J. Integr. Plant Biol. 2012, 54, 422–429. [Google Scholar] [CrossRef] [Scilit]
  58. Tian, J.; Cheng, L.; Han, Z.-Y.; Yao, Y.-C. Tobacco rattle virus mediated gene silencing in strawberry plants. Plant Cell Tissue Organ Cult. (PCTOC) 2014, 120, 1131–1138. [Google Scholar] [CrossRef] [Scilit]
  59. Zhang, J.; Yu, D.; Zhang, Y.; Liu, K.; Xu, K.; Zhang, F.; Wang, J.; Tan, G.; Nie, X.; Ji, Q.; et al. Vacuum and co-cultivation Agroinfiltration of (Germinated) seeds results in tobacco rattle virus (TRV) mediated Whole-Plant Virus-Induced Gene Silencing (VIGS) in wheat and maize. Front. Plant Sci. 2017, 8, 393. [Google Scholar] [CrossRef] [Scilit]
  60. Brigneti, G.; Martín-Hernández, A.M.; Jin, H.; Chen, J.; Baulcombe, D.C.; Baker, B.; Jones, J.D.G. Virus-induced gene silencing in Solanum species. Plant J. 2004, 39, 264–272. [Google Scholar] [CrossRef] [Scilit]
  61. Matsuo, K.; Hong, J.-S.; Tabayashi, N.; Ito, A.; Masuta, C.; Matsumura, T. Development of Cucumber mosaic virus as a vector modifiable for different host species to produce therapeutic proteins. Planta 2006, 225, 277–286. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  62. González, I.; Martínez, L.; Rakitina, D.V.; Lewsey, M.G.; Atencio, F.A.; Llave, C.; Kalinina, N.O.; Carr, J.P.; Palukaitis, P.; Canto, T. Cucumber Mosaic Virus 2B Protein subcellular targets and interactions: Their significance to RNA silencing suppressor activity. Mol. Plant-Microbe Interact. 2010, 23, 294–303. [Google Scholar] [CrossRef] [Scilit]
  63. Duan, C.-G.; Fang, Y.-Y.; Zhou, B.-J.; Zhao, J.-H.; Hou, W.-N.; Zhu, H.; Ding, S.-W.; Guo, H.-S. Suppression of Arabidopsis ARGONAUTE1-Mediated Slicing, Transgene-Induced RNA Silencing, and DNA Methylation by Distinct Domains of the Cucumber mosaic virus 2b Protein. Plant Cell 2012, 24, 259–274. [Google Scholar] [CrossRef] [Scilit]
  64. Takeshita, M.; Koizumi, E.; Noguchi, M.; Sueda, K.; Shimura, H.; Ishikawa, N.; Matsuura, H.; Ohshima, K.; Natsuaki, T.; Kuwata, S.; et al. Infection Dynamics in Viral Spread and Interference Under the Synergism Between Cucumber mosaic virus and Turnip mosaic virus. Mol. Plant-Microbe Interact. 2011, 25, 18–27. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  65. Liao, Q.; Tu, Y.; Carr, J.P.; Du, Z. An improved cucumber mosaic virus-based vector for efficient decoying of plant microRNAs. Sci. Rep. 2015, 5, 13178. [Google Scholar] [CrossRef] [Scilit]
  66. Kong, L.J. A geminivirus replication protein interacts with the retinoblastoma protein through a novel domain to determine symptoms and tissue specificity of infection in plants. EMBO J. 2000, 19, 3485–3495. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  67. Chellappan, P.; Vanitharani, R.; Ogbe, F.; Fauquet, C.M. Effect of temperature on Geminivirus-Induced RNA silencing in plants. Plant Physiol. 2005, 138, 1828–1841. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  68. Rajabu, C.A.; Dallas, M.M.; Chiunga, E.; De León, L.; Ateka, E.M.; Tairo, F.; Ndunguru, J.; Ascencio-Ibanez, J.T.; Hanley-Bowdoin, L. SEGS-1 a cassava genomic sequence increases the severity of African cassava mosaic virus infection in Arabidopsis thaliana. Front. Plant Sci. 2023, 14, 1250105. [Google Scholar] [CrossRef] [Scilit]
  69. Lentz, E.M.; Kuon, J.-E.; Alder, A.; Mangel, N.; Zainuddin, I.M.; McCallum, E.J.; Anjanappa, R.B.; Gruissem, W.; Vanderschuren, H. Cassava geminivirus agroclones for virus-induced gene silencing in cassava leaves and roots. Plant Methods 2018, 14, 73. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  70. Ju, Z.; Cao, D.; Gao, C.; Zuo, J.; Zhai, B.; Li, S.; Zhu, H.; Fu, D.; Luo, Y.; Zhu, B. A Viral Satellite DNA Vector (TYLCCNV) for functional analysis of miRNAs and SIRNAs in plants. Plant Physiol. 2017, 173, 1940–1952. [Google Scholar] [CrossRef] [Scilit]
  71. Gosselé, V.; Faché, I.; Meulewaeter, F.; Cornelissen, M.; Metzlaff, M. SVISS—A novel transient gene silencing system for gene function discovery and validation in tobacco plants. Plant J. 2002, 32, 859–866. [Google Scholar] [CrossRef] [Scilit]
  72. Ju, Z.; Wang, L.; Cao, D.; Zuo, J.; Zhu, H.; Fu, D.; Luo, Y.; Zhu, B. A viral satellite DNA vector-induced transcriptional gene silencing via DNA methylation of gene promoter in Nicotiana benthamiana. Virus Res. 2016, 223, 99–107. [Google Scholar] [CrossRef] [Scilit]
  73. Wang, R.; Yang, X.; Wang, N.; Liu, X.; Nelson, R.S.; Li, W.; Fan, Z.; Zhou, T. An efficient virus-induced gene silencing vector for maize functional genomics research. Plant J. 2016, 86, 102–115. [Google Scholar] [CrossRef] [Scilit]
  74. Liu, E.; Page, J.E. Optimized cDNA libraries for virus-induced gene silencing (VIGS) using tobacco rattle virus. Plant Methods 2008, 4, 5. [Google Scholar] [CrossRef] [Scilit]
  75. Hartl, M.; Merker, H.; Schmidt, D.D.; Baldwin, I.T. Optimized virus-induced gene silencing in Solanum nigrum reveals the defensive function of leucine aminopeptidase against herbivores and the shortcomings of empty vector controls. New Phytol. 2008, 179, 356–365. [Google Scholar] [CrossRef] [Scilit]
  76. Mardini, M.; Kazancev, M.; Ivoilova, E.; Utkina, V.; Vlasova, A.; Demurin, Y.; Soloviev, A.; Kirov, I. Advancing virus-induced gene silencing in sunflower: Key factors of VIGS spreading and a novel simple protocol. Plant Methods 2024, 20, 122. [Google Scholar] [CrossRef] [Scilit]
  77. Yuan, C.; Li, C.; Yan, L.; Jackson, A.O.; Liu, Z.; Han, C.; Yu, J.; Li, D. A high throughput barley stripe mosaic virus vector for virus induced gene silencing in monocots and dicots. PLoS ONE 2011, 6, e26468. [Google Scholar] [CrossRef] [Scilit]
  78. Meng, L.-H.; Wang, R.-H.; Zhu, B.-Z.; Zhu, H.-L.; Luo, Y.-B.; Fu, D.-Q. Efficient Virus-Induced Gene Silencing in Solanum rostratum. PLoS ONE 2016, 11, e0156228. [Google Scholar] [CrossRef] [Scilit]
  79. Ryu, C.; Anand, A.; Kang, L.; Mysore, K.S. Agrodrench: A novel and effective agroinoculation method for virus-induced gene silencing in roots and diverse Solanaceous species. Plant J. 2004, 40, 322–331. [Google Scholar] [CrossRef] [Scilit]
  80. He, G.; Zhao, X.; Xu, Y.; Wang, Y.; Zhang, Z.; Xiao, L.; Hudson, M.; Hu, R.; Li, S. An efficient virus-induced gene silencing (VIGS) system for gene functional studies in Miscanthus. GCB Bioenergy 2023, 15, 805–820. [Google Scholar] [CrossRef] [Scilit]
  81. Fu, D.-Q.; Zhu, B.-Z.; Zhu, H.-L.; Zhang, H.-X.; Xie, Y.-H.; Jiang, W.-B.; Zhao, X.-D.; Luo, Y.-B. Enhancement of virus-induced gene silencing in tomato by low temperature and low humidity. Mol. Cells 2006, 21, 153–160. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  82. Fei, Y.; Pyott, D.E.; Molnar, A. Temperature modulates virus-induced transcriptional gene silencing via secondary small RNAs. New Phytol. 2021, 232, 356–371. [Google Scholar] [CrossRef] [Scilit]
  83. Szittya, G. Low temperature inhibits RNA silencing-mediated defence by the control of siRNA generation. EMBO J. 2003, 22, 633–640. [Google Scholar] [CrossRef] [Scilit]
  84. Burch-Smith, T.M.; Schiff, M.; Liu, Y.; Dinesh-Kumar, S.P. Efficient Virus-Induced Gene Silencing in Arabidopsis. Plant Physiol. 2006, 142, 21–27. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  85. Pumplin, N.; Voinnet, O. RNA silencing suppression by plant pathogens: Defence, counter-defence and counter-counter-defence. Nat. Rev. Microbiol. 2013, 11, 745–760. [Google Scholar] [CrossRef] [Scilit]
  86. Pinczés, D.; Sáray, R.; Nemes, K.; Palkovics, L.; Salánki, K. Viral coat proteins decrease the gene silencing activity of cognate and heterologous viral suppressors. Sci. Rep. 2024, 14, 31008. [Google Scholar] [CrossRef] [Scilit]
  87. Zhou, T.; Murphy, A.M.; Lewsey, M.G.; Westwood, J.H.; Zhang, H.-M.; González, I.; Canto, T.; Carr, J.P. Domains of the cucumber mosaic virus 2b silencing suppressor protein affecting inhibition of salicylic acid-induced resistance and priming of salicylic acid accumulation during infection. J. Gen. Virol. 2014, 95, 1408–1413. [Google Scholar] [CrossRef] [Scilit]
  88. Westwood, J.H.; Lewsey, M.G.; Murphy, A.M.; Tungadi, T.; Bates, A.; Gilligan, C.A.; Carr, J.P. Interference with jasmonic acid-regulated gene expression is a general property of viral suppressors of RNA silencing but only partly explains virus-induced changes in plant–aphid interactions. J. Gen. Virol. 2013, 95, 733–739. [Google Scholar] [CrossRef] [Scilit]
  89. García, A.; Aragonés, V.; Gioiosa, S.; Herraiz, F.J.; Ortiz-García, P.; Prohens, J.; Daròs, J.-A.; Pasin, F. Comparative genomics-driven design of virus-delivered short RNA inserts triggering robust gene silencing. bioRxiv 2025, 1–3. [Google Scholar] [CrossRef] [Scilit]
  90. Zhang, Z.; Li, D.-W.; Jin, J.-H.; Yin, Y.-X.; Zhang, H.-X.; Chai, W.-G.; Gong, Z.-H. VIGS approach reveals the modulation of anthocyanin biosynthetic genes by CaMYB in chili pepper leaves. Front. Plant Sci. 2015, 6, 500. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  91. Kim, J.; Park, M.; Jeong, E.S.; Lee, J.M.; Choi, D. Harnessing anthocyanin-rich fruit: A visible reporter for tracing virus-induced gene silencing in pepper fruit. Plant Methods 2017, 13, 3. [Google Scholar] [CrossRef] [Scilit]
  92. Byun, J.; Kim, T.-G.; Lee, J.-H.; Li, N.; Jung, S.; Kang, B.-C. Identification of CaAN3 as a fruit-specific regulator of anthocyanin biosynthesis in pepper (Capsicum annuum). Theor. Appl. Genet. 2022, 135, 2197–2211. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  93. Sarde, S.J.; Bouwmeester, K.; Venegas-Molina, J.; David, A.; Boland, W.; Dicke, M. Involvement of sweet pepperCaLOX2in jasmonate-dependent induced defence against Western flower thrips. J. Integr. Plant Biol. 2018, 61, 1085–1098. [Google Scholar] [CrossRef] [Scilit]
  94. Chen, R.; Ma, J.; Luo, D.; Hou, X.; Ma, F.; Zhang, Y.; Meng, Y.; Zhang, H.; Guo, W. CaMADS, a MADS-box transcription factor from pepper, plays an important role in the response to cold, salt, and osmotic stress. Plant Sci. 2018, 280, 164–174. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  95. Wang, J.-E.; Liu, K.-K.; Li, D.-W.; Zhang, Y.-L.; Zhao, Q.; He, Y.-M.; Gong, Z.-H. A Novel Peroxidase CanPOD Gene of Pepper Is Involved in Defense Responses to Phytophtora capsici Infection as well as Abiotic Stress Tolerance. Int. J. Mol. Sci. 2013, 14, 3158–3177. [Google Scholar] [CrossRef] [Scilit]
  96. Cheng, Y.; Ahammed, G.J.; Yao, Z.; Ye, Q.; Ruan, M.; Wang, R.; Li, Z.; Zhou, G.; Wan, H. Comparative genomic analysis reveals extensive genetic variations of WRKYs in solanaceae and functional variations of CAWRKYs in pepper. Front. Genet. 2019, 10, 492. [Google Scholar] [CrossRef] [Scilit]
  97. Zhang, Y.-L.; Jia, Q.-L.; Li, D.-W.; Wang, J.-E.; Yin, Y.-X.; Gong, Z.-H. Characteristic of the Pepper CaRGA2 Gene in Defense Responses against Phytophthora capsici Leonian. Int. J. Mol. Sci. 2013, 14, 8985–9004. [Google Scholar] [CrossRef] [Scilit]
  98. Noman, A.; Hussain, A.; Adnan, M.; Khan, M.I.; Ashraf, M.F.; Zainab, M.; Khan, K.A.; Ghramh, H.A.; He, S. A novel MYB transcription factor CaPHL8 provide clues about evolution of pepper immunity againstsoil borne pathogen. Microb. Pathog. 2019, 137, 103758. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  99. Chung, E.; Ryu, C.; Oh, S.; Kim, R.N.; Park, J.M.; Cho, H.S.; Lee, S.; Moon, J.S.; Park, S.; Choi, D. Suppression of pepperSGT1andSKP1causes severe retardation of plant growth and compromises basal resistance. Physiol. Plant. 2006, 126, 605–617. [Google Scholar] [CrossRef] [Scilit]
  100. Jin, J.-H.; Zhang, H.-X.; Tan, J.-Y.; Yan, M.-J.; Li, D.-W.; Khan, A.; Gong, Z.-H. A New Ethylene-Responsive Factor CaPTI1 Gene of Pepper (Capsicum annuum L.) Involved in the Regulation of Defense Response to Phytophthora capsici. Front. Plant Sci. 2016, 6, 1217. [Google Scholar] [CrossRef] [Scilit]
  101. Wei, X.; Meng, C.; Yuan, Y.; Nath, U.K.; Zhao, Y.; Wang, Z.; Yang, S.; Li, L.; Niu, L.; Yao, Q.; et al. CaPSY1 gene plays likely the key role in carotenoid metabolism of pepper (Capsicum annuum) at ripening. Funct. Plant Biol. 2020, 48, 141. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  102. Song, Y.; Cheng, Q.; Li, X.; Ma, S.; Shen, H.; Sun, L. The MADS-Box Transcription Factor CaRIN Positively Regulates Chlorophyll Degradation During Pepper (Capsicum annuum L.) Fruit Ripening by Repressing the Expression of CaLhcb-P4. Plants 2025, 14, 445. [Google Scholar] [CrossRef] [Scilit]
  103. Cheng, Q.; Li, T.; Ai, Y.; Lu, Q.; Wang, Y.; Wu, L.; Liu, J.; Sun, L.; Shen, H. Phenotypic, genetic, and molecular function of msc-2, a genic male sterile mutant in pepper (Capsicum annuum L.). Theor. Appl. Genet. 2019, 133, 843–855. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  104. Venkatesh, J.; Kang, M.-Y.; Liu, L.; Kwon, J.-K.; Kang, B.-C. F-Box Family Genes, LTSF1 and LTSF2, Regulate Low-Temperature Stress Tolerance in Pepper (Capsicum chinense). Plants 2020, 9, 1186. [Google Scholar] [CrossRef] [Scilit]
  105. Gou, B.; Duan, P.; Wei, M.; Zhao, S.; Wang, Y.; Yang, N.; Zhang, G.; Wei, B. Silencing CATPS1 increases the sensitivity to low temperature and salt stresses in pepper. Agronomy 2023, 13, 319. [Google Scholar] [CrossRef] [Scilit]
  106. Miki, D.; Itoh, R.; Shimamoto, K. RNA silencing of single and multiple members in a gene family of rice. Plant Physiol. 2005, 138, 1903–1913. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. The generalized scheme of VIGS technology. The process begins with the cloning of a target gene fragment into a viral vector (1) and its transformation into Agrobacterium tumefaciens (2). This is followed by the cultivation of agrobacteria on solid (3) and in liquid nutrient media (4–6) to obtain a working infiltration buffer. The plant is inoculated via agroinfiltration (7), which ultimately leads to the systemic silencing of the target gene and the emergence of expected phenotypic changes (8).
Horticulturae 11 01297 g001
Figure 2. The structure of the viral vector TRV1 and TRV2. LB and RB are the left and right borders of the vector, p35s*2 is the double promoter of the 35S, RdRp is an RNA-dependent RNA polymerase, MP is a motor protein, 16K is an RNA interference suppressor, T is a terminator, Rz is a self-cleavable ribozyme, CP is a coat protein (coat protein), MCS is a multiple cloning site.
Horticulturae 11 01297 g002
Figure 3. Structure of the BBWV2 viral vector. LB and RB are the left and right borders of the vector, p35s*2 is the double promoter of the 35S, Co-Pro is a protease cofactor, NTBM is an NTP-binding motif, VPg is a protein associated with the viral genome, Pro is a protease, RdRp is an RNA-dependent RNA polymerase, Rz is a self-cleaving ribozyme, T is a terminator, MP is a motor protein, LCP is a large envelope protein, SCP is a small envelope protein, and GOI is a gene of interest.
Horticulturae 11 01297 g003
Figure 4. Structure of the CMV viral vector. LB and RB are the left and right borders of the vector, p35s*2 is the double promoter of the 35S, 1a, 2a, 2b* are specific proteins, MP is the motor protein, CP is the envelope protein, MCS is the multiple cloning site, Rz is the self-cleaving ribozyme, T is the terminator. Proteins 1a and 2a are involved in viral replication; 2b has the activity of suppressor of RNA silencing, control of basal resistance of the host organism and is the object of deletion during vector construction.
Horticulturae 11 01297 g004
Figure 5. Structure of the CLCrV viral vector. LB and RB are the left and right borders of the vector. CR (common region) contains the regulatory elements for viral replication and translation. AV1 is a coat protein (CP), AC1 is the replication protein, AC2 is the transcription protein, AC3 is the replication enhancer protein, AC4 is viral suppressor of RNA silencing (VSR) and MCS is the multiple cloning site. BV1 is a nuclear-shuttle protein for transporting viral ssDNA in and out of the cell nucleus, BC1 is a movement protein for moving the viral vector through the plasmodesmus, HygR is a hygromycin resistance protein.
Horticulturae 11 01297 g005
Figure 6. Structure of the ACMV viral vector used in VIGS. LB and RB are the left and right borders of the vector. CR is a common region, containing the regulatory elements for viral replication and translation, AV1 is a coat protein (CP), AV2 is an RNAi suppressor protein, AC1 is a replication protein, AC2 is a transcription protein, AC3 is a replication enhancer protein, AC4 is viral suppressor of RNA silencing (VSR), and MCS is a multiple cloning site. BV1 is a nuclear-shuttle protein for transporting viral ssDNA in and out of the cell nucleus, BC1 is a movement protein essential for the viral vector transportation through the plasmodesmus.
Horticulturae 11 01297 g006
Figure 7. Methods of viral vector delivery. As an example, the recombinant vector contains a fragment of the phytoene desaturase gene (PDS). (A). Leaf infiltration (injection)—a suspension of agrobacteria containing viral vectors is injected into the dorsal side of the plant using a syringe without a needle. The suspension penetrates into the intercellular substance and spreads through the leaf. (B). Spraying of the inoculum is carried out using a spray gun and helps to reach an extensive field of infection, however, this method does not ensure full penetration of viral vectors, since it is sprayed only on the surface of the plant. (C). Agrodrench involves the introduction of a suspension of agrobacteria through the soil adjacent to the roots of the plant, which allows for the use of methods for young shoots that do not have sufficient leaf size for infiltration with a syringe. (D). Agroinjection of fruits applies the same principle as leaf infiltration to study gene function during fruit development, with injections being administered directly into young, developing fruits. (E). Soaking seeds or plant sprouts under vacuum infiltration conditions. (F). Secondary infiltration. Before inoculation of the test plant, the primary plant is inoculated (primary infiltration). After the symptoms appear, the leaf with the viral vector is homogenized, and the resulting mixture infects the test plant (secondary infiltration). It is used on monocotyledonous plants.
Horticulturae 11 01297 g007
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.