Review

Bioactive Compounds from Edible Mushrooms as Pharmaceutical Ingredients: A Comprehensive Review of the Developmental Pipeline


by
Samuel Oluwasegun Adesida
1,
Ridwan Abiola Oyetunji
2 and
Chibuisi Gideon Alimba
3,*
1
West African Science Service Centre on Climate Change and Adapted Land Use (WASCAL), Graduate Research Program in Climate Change and Biodiversity, Université Felix Houphouet-Boigny, Abidjan P.O. Box 582, Côte d’Ivoire
2
Department of Botany, University of Ibadan, Ibadan 200001, Nigeria
3
Leibniz Research Centre for Working Environment and Human Factors (IfADo), Technical University of Dortmund, 44139 Dortmund, Germany
*
Author to whom correspondence should be addressed.
Processes 2026, 14(5), 795; https://doi.org/10.3390/pr14050795
Submission received: 24 January 2026 / Revised: 20 February 2026 / Accepted: 26 February 2026 / Published: 28 February 2026

Abstract

Edible mushrooms have long been valued as functional foods and traditional remedies, yet a significant developmental gap hinders their transition from nutraceuticals to standardized pharmaceutical ingredients. This narrative review provides a comprehensive and integrative analysis of edible mushroom-derived bioactive compounds as emerging candidates for pharmaceutical development. It examines major chemical classes, including polysaccharides (e.g., β-glucans), proteins (e.g., lectins, FIPs), triterpenoids (e.g., ganoderic acids), nucleosides (e.g., adenosine and cordycepin), and phenolic compounds, which underpin immunomodulatory, anticancer, antioxidant, anti-inflammatory, and metabolic activities. Beyond bioactivity, the review critically examines the downstream processing pipeline required for translation into pharmaceutical ingredients, encompassing controlled biomass production, pre-extraction processing, extraction technologies, isolation and purification strategies, and structural elucidation techniques. Key bottlenecks are identified, including bioavailability limitations of β-glucans (2–5%), lack of standardization, limited human clinical evidence, and regulatory constraints, explaining why robust preclinical evidence has not consistently translated into clinical success. Emerging solutions are also highlighted, including application of multi-omics tools, nano-encapsulation strategies, and synthetic biology approaches to improve scalability and reproducibility. By synthesizing research on natural product chemistry, biotechnology, and pharmacology, this study maps the journey of edible mushrooms from traditional dietary components to pharmaceutical-grade ingredients, providing a focused resource for researchers and industry stakeholders aiming to navigate mushroom-based drug development.

1. Introduction

Edible mushrooms, with an estimated 3000 documented species, represent one of the most widely recognized edible forest products worldwide [1]. Their long-standing culinary relevance across diverse cultures is attributed to their distinctive flavor, aroma, and texture [2]. Historically, mushrooms were valued as both food and therapeutic resources long before their bioactive properties were scientifically understood. Ancient civilizations, including the Romans and Greeks, regularly incorporated mushrooms into their diets, while others revered them as potent medicinal agents. For instance, certain species were referred to as the “elixir of life” in China and the “flesh of the gods” in Egypt [3,4]. Although mycotherapy has been deeply rooted in Asian traditional medicine for millennia, its adoption in Western countries has gained momentum only in recent decades [5].
The intersection of edibility and medicinal value in mushrooms is well established, as many edible species exhibit pharmacological properties, and several renowned medicinal mushrooms are regularly consumed as part of the diet [2]. The health-enhancing effects of edible mushrooms, observed since antiquity, are now attributed to the bioactivity of their secondary metabolites, including polysaccharides, polyphenols, proteins, terpenes, and terpenoids. The literature has documented a wide array of pharmacological activities for these bioactive compounds, including anticancer, antioxidant, hepatoprotective, immunomodulatory and antimicrobial effects [6]. Consequently, edible mushrooms have become a significant source of active ingredients for nutraceutical and pharmaceutical formulations [3]. Notably, the spores and basidiocarps of Ganoderma lucidum, a globally renowned edible and medicinal mushroom, are processed into tablets, injectables, and soft-gel capsules for various therapeutic purposes [7]. Likewise, nutraceuticals derived from edible mushrooms represent an expanding segment of the overall dietary supplement market [8].
Growing recognition of the therapeutic value of edible mushrooms has intensified their demand among consumers and pharmaceutical industries alike. While whole mushroom biomass can be consumed directly, its bioactive constituents can also be isolated and formulated into novel pharmaceutical products. This increased demand has subsequently stimulated the expansion of commercial cultivation and global market of edible mushrooms [9]. Global mushroom production, for instance, increased 15.6-fold between 1990 and 2022 [10]. Also, the global mushroom market is projected to rise from USD 48.8 billion in 2022 to USD 83.5 billion by 2030, at an annual rate of 7% [11]. These commercialization trends highlight the growing opportunity to harness edible mushrooms as sources of natural-based pharmaceutical ingredients.
Although several synthetic drugs exist and are currently in use for disease management, concerns over unfavorable side effects and inconsistent therapeutic outcomes have renewed interest in natural product-based drug discovery [2,12]. Consequently, recent research efforts increasingly target the extraction and purification of mushroom-derived bioactive compounds for pharmaceutical development. For example, quercetin, a flavonol present in some edible mushrooms, is utilized pharmaceutically to regulate blood glucose and enhance insulin sensitivity [13]. Similarly, a biocompatible antioxidant and anti-inflammatory hydrogel developed for diabetic wound healing incorporates G. lucidum polysaccharide (GLP) [14]. Such bioactive molecules provide complementary therapeutic benefits alongside conventional drugs, often enhancing efficacy while lowering side effects [12]. Furthermore, the fruiting bodies, cultured mycelia, and fermentation broths of edible mushrooms are increasingly being recognized as rich reservoirs of novel active compounds. Their attractiveness to pharmaceutical industries is additionally supported by favorable cultivation characteristics, including rapid growth, high biomass yield, and modest space requirements [15].
Despite compelling evidence supporting the bioactivities and pharmacological potential of edible mushrooms, their development pathway into standardized, pharmaceutical-grade raw materials remains poorly integrated. Critical downstream processing stages, such as scalable production, standardized extraction and isolation, and comprehensive molecular characterization, are often addressed in isolation rather than as a unified framework. This knowledge gap may hinder clinical testing and wide-scale therapeutic applications [5]. Accordingly, this comprehensive review elucidates how edible mushrooms are transcending their traditional nutraceutical roles to emerge as viable candidates for modern pharmaceutical development. It synthesizes current knowledge to provide a systematic overview of the multifaceted development pathway, focusing on the major downstream procedures essential for transforming mushroom bioactive compounds into high-purity, reliable pharmaceutical ingredients.
Moreover, unlike previous reviews that have predominantly concentrated on bioactivity cataloging, single mushroom species and/or isolated classes of compounds [16,17,18,19,20], the present review provides a holistic and explicitly translational synthesis of mushroom-derived bioactives. By systematically integrating chemical diversity with extraction and purification strategies, structural elucidation, and pharmaceutical development constraints across multiple edible mushroom taxa, this work bridges natural product chemistry with practical drug development considerations. Importantly, this integrative perspective moves beyond descriptive accounts of bioactivity to critically examine how mushroom bioactives can be rationally prioritized, optimized, and advanced within realistic pharmaceutical development pipelines. To establish their basis for pharmaceutical consideration, the review links the chemical diversity of bioactive constituents in edible mushrooms with their associated biological activities, thereby elucidating the mechanistic basis of their therapeutic potential. It further highlights key translational challenges that connect molecular characterization with the practical requirements for clinical and industrial implementation.

2. Methodology for the Narrative Review

To develop this narrative review, relevant literature was identified through searches of major scientific databases, including Google Scholar, PubMed, Scopus, Web of Science, ScienceDirect, and the Directory of Open Access Journals (DOAJ). Priority was given to studies published between 2020 and 2026 in order to capture recent advances in the development, extraction, and pharmaceutical utilization of bioactive compounds from edible mushrooms. The search strategy employed the core keywords “edible mushrooms” and “bioactive compounds”, combined with other related terms such as cultivation, solid state fermentation, submerged liquid fermentation, extraction, isolation, purification, characterization, standardization and specific pharmacological activities (e.g., anticancer, antimicrobial, antioxidant, neuroprotective, and cardiovascular effects). Moreover, the reference lists of the retrieved articles were manually screened to identify additional relevant studies that were not captured through the electronic database searches. Literature retrieval was completed in 10 January 2026. Following the initial search, duplicate records were removed, and non-English publications were excluded. Studies focusing primarily on other natural product sources, such as medicinal plants, were also excluded. Relevant titles and abstracts were examined to identify studies aligned with the thematic scope of this review, with emphasis placed on studies addressing the biological activities of mushroom-derived bioactive compounds and/or downstream processing aspects pertinent to their pharmaceutical development. Full-text articles were subsequently reviewed and included only if they provided substantive information on edible mushrooms and their bioactive constituents in relation to the predefined thematic scope. The final body of literature (n = 199) comprised original research articles, review papers, institutional/technical reports and relevant book chapters. These sources were qualitatively synthesized to provide an integrated and critical narrative overview of the role of edible mushroom bioactives in pharmaceutical innovation. In this review, the term “bioactive compounds or bioactives” is used as an umbrella descriptor for mushroom-derived molecules exhibiting biological activity, while “secondary metabolites” refers specifically to low-molecular-weight fungal metabolites. The term “pharmaceutical ingredients” is reserved for compounds or standardized extracts considered within a drug-development or regulatory framework.

3. Chemistry and Bioactivity: The Pharmaceutical Basis of Mushroom Compounds

The therapeutic potential of edible mushrooms is primarily attributed to a diverse array of bioactive compounds, which can be broadly categorized into high-molecular-weight macromolecules and low-molecular-weight secondary metabolites, each defined by distinct chemical characteristics and biological functions [21]. High-molecular-weight compounds, including polysaccharides, proteins, and nucleic acid–protein complexes, are predominantly associated with immunomodulatory, antitumor, and antioxidant activities. In contrast, low-molecular-weight metabolites such as terpenoids, sterols, polyphenols, and related secondary compounds largely contribute to antioxidant, anticancer, antiviral, anti-inflammatory, immune-modulating and cardioprotective effects [22].
Importantly, these chemical classes do not act in isolation; rather, their structural features determine molecular mechanisms and pharmacological effects. The abundance and composition of these bioactive constituents vary considerably among mushroom species and are strongly influenced by cultivation substrates, environmental and fruiting conditions (cultivated versus wild), and developmental stage [2,21]. For example, Barros et al. [23] reported markedly higher flavonoid concentrations (16.56 mg/g) in wild-harvested species of Agaricus, Lentinus, and Pleurotus. Conversely, cultivated counterparts of the same genera were found to contain low or undetectable levels of certain phenolic compounds, including flavonoids and lignans [24], underscoring the impact of growth conditions on phytochemical profiles and, by extension, bioactivity.

3.1. High-Molecular-Weight Bioactive Compounds

High-molecular-weight bioactive constituents in edible mushrooms play a central role in mediating many of the health-promoting properties associated with edible mushrooms, particularly those related to immune modulation, tumor suppression, and host defense. Notwithstanding, from a pharmaceutical perspective, the structural complexity and molecular weight of these compounds present challenges related to oral bioavailability, batch consistency, and regulatory definition of an active pharmaceutical ingredient (API). These features necessitate advanced formulation strategies and robust analytical standardization prior to clinical translation.

3.1.1. Polysaccharides

Polysaccharides occur widely in nature, including in plants and microbial extracellular polymeric substances [25]. Among these, mushroom-derived polysaccharides have attracted substantial interest due to their demonstrated relevance in molecular biology, immunology, biotechnology, and pharmaceutical sciences [26]. Compared with polysaccharides from other biological sources, those isolated from mushrooms exhibit remarkable structural diversity, reflected in variations in molecular weight, monosaccharide composition, degree of branching, chain length, and three-dimensional conformation [27]. The strong dependence of polysaccharide bioactivity on these structural features highlights structural elucidation as a prerequisite for reproducible pharmacological outcomes. Mushroom polysaccharides are predominantly composed of α- and/or β-glucans, with β-glucans representing the principal bioactive fraction. These β-glucans constitute one of the two major structural components of the fungal cell wall, alongside chitin [9]. Common glycosidic linkages include (1→3)-β-D-glucan, (1→6)-β-D-glucan, (1→3)-α-D-glucan, and mixed-linkage structures, reflecting substantial molecular heterogeneity [28,29].
Functionally, β-glucans elicit a broad spectrum of biological responses, including immunomodulatory, antitumor, antioxidant, and anti-inflammatory effects, primarily through interactions with pattern-recognition receptors on immune cells [30]. Chan et al. [31], for instance, demonstrated that β-glucans mediate antimicrobial immune responses via specific receptors such as dectin-1, complement receptor 3 (CR3), and Toll-like receptors 2 and 6 (TLR2/6). Sulfated β-glucans from Agaricus brasiliensis have further been shown to prevent HSV-1 and HSV-2 viral entry at low microgram concentrations, highlighting their antiviral potential [32].
Notable examples of bioactive mushroom-derived β-glucans include schizophyllan from Schizophyllum commune, lentinan from Lentinula edodes, pleuran from Pleurotus spp., calocyban from Calocybe indica and the Maitake D-fraction from Grifola frondosa [2,9]. Several of these polysaccharides have demonstrated tumor growth inhibition through activation of macrophages, natural killer (NK) cells, and cytokine (TNF-α, IL-2, and IFN-γ) production, reinforcing their relevance in cancer immunotherapy [33,34]. In addition to homopolysaccharides, mushrooms also contain heteropolysaccharides, such as xylomannans and branched glucans, which further expand their functional repertoire [30].
Polysaccharides may also associate with other biomolecules through covalent or non-covalent interactions to form bioactive complexes, among which polysaccharide–protein complexes (PPCs) are particularly prominent. Well-known examples include Krestin and Coriolan isolated from Trametes versicolor, both comprising β-glucans conjugated to protein moieties [1]. These complexes have been shown to promote macrophage polarization toward tumor-suppressive M1 phenotype, reducing immunosuppressive cytokines and enhancing antitumor immunity [35]. Similarly, Agaricus spp. produces biologically active PPCs characterized by protein-bound β-(1→6)-glucan structures, which have been linked to pronounced immunomodulatory and anticancer effects [31].

3.1.2. Nucleic Acids and Nucleosides

Nucleic acids and their derivatives, including nucleobases, nucleosides, and nucleotides, are essential biomolecules involved in cellular metabolism, gene regulation, and intracellular signaling [36,37]. Edible mushrooms represent a rich dietary source of these compounds, containing purine and pyrimidine nucleobases (e.g., adenine, guanine, uracil, and cytosine), nucleosides (e.g., adenosine, guanosine, uridine, cytidine, thymidine, and inosine), and nucleotides such as adenosine monophosphate (AMP) and guanosine monophosphate (GMP) [37]. Distinct mushroom species exhibit characteristic nucleoside profiles. For example, Agaricus bisporus and Morchella deliciosa are enriched in adenosine, guanosine, xanthosine, and uridine [38], whereas inosine, cytidine, thymidine, and cordycepin have been reported in Antrodia camphorata, Agrocybe aegerita, and Tricholoma matsutake [39,40]. Several mushroom-derived nucleosides, notably adenosine and cordycepin, have been implicated in antidiabetic activities. In particular, cordycepin from Cordyceps spp. has been shown to modulate the expression of diabetes-associated genes by attenuating nitric oxide (NO) production and pro-inflammatory cytokine release through suppression of NF-κB-dependent inflammatory signaling pathways [41]. This modulation is associated with reduced expression of key inflammatory mediators, including IL-1β, IL-6, and TNF-α, as well as the downregulation of upstream regulators such as Toll-like receptor 4 (TLR4) and myeloid differentiation primary response protein 88 (MyD88) [42]. These nucleoside constituents therefore contribute meaningfully to the immunoregulatory, neuroprotective and tissue-repair activities associated with edible mushrooms [37].

3.1.3. Proteins and Peptides

Proteins and peptides are another major class of bioactive constituents in edible mushrooms, contributing significantly to their nutritional and therapeutic value. Protein content varies widely among species. Notably, Hericium erinaceus (Lion’s Mane), Ophiocordyceps sinensis (Cordyceps), and L. edodes (Shiitake) are particularly protein-rich, often exceeding 20% protein content [30]. Mushroom-derived proteins and peptides have been linked to a broad spectrum of biological activities, including hypotensive and angiotensin-converting enzyme (ACE) inhibitory effects, antioxidant, anticancer, antiviral, and antibacterial properties [43]. The major classes of bioactive fungal proteins include lectins, fungal immunomodulatory proteins (FIPs), and enzymatic proteins such as nucleases, ribonucleases, and laccases [44]. Lectins, also known as glycoproteins, exert their biological effects by interacting with specific sugar residues, leading to agglutination and modulation of immune responses. These interactions have been associated with enhanced insulin secretion, glycemic control, immune stimulation, and chemopreventive effects [1,45]. For instance, investigations into lectins and proteins across Cantharellus cibarius, Imleria badia, Lactarius deliciosus, and Boletus edulis have indicated immunoregulatory activity, including enhanced Th1 lymphocyte responses and suppression of COX-2 and prostaglandin synthesis [46].
Fungal immunomodulatory proteins represent another distinctive group of mushroom proteins with the ability to selectively target immune cells. These proteins have been identified in species such as Flammulina velutipes and several Ganoderma spp. [9]. Notable examples include GMI from Ganoderma microsporum, Fip-gts from G. tsugae, and Ling Zhi-8 from G. lucidum, all of which exhibit antimetastatic and immunoregulatory activities [47,48,49]. Purified and structurally characterized protein fractions from Pleurotus eryngii were shown to suppress tumor cell proliferation in a dose-dependent manner, further highlighting the pharmaceutical relevance of mushroom-derived proteins as natural antitumor agents with additional immunostimulatory properties [50].
In addition, low-molecular-weight peptides such as cordymin, isolated from Cordyceps spp., have demonstrated the ability to reduce blood glucose and glycated hemoglobin levels while alleviating oxidative stress in diabetic animal models [51]. Ribonucleases, which induce apoptosis through RNA degradation, have also been shown to exhibit antibacterial activity against clinically relevant pathogens, including Staphylococcus aureus and Pseudomonas aeruginosa [52]. Edible mushrooms also provide a rich source of essential and non-essential amino acids, including glutamic acid, aspartic acid, arginine, ornithine, and γ-aminobutyric acid (GABA), further enhancing their functional and therapeutic relevance [44].

3.2. Low-Molecular-Weight Bioactive Compounds

Low-molecular-weight bioactive compounds isolated from edible mushrooms primarily function as secondary metabolites and are generally more readily absorbed than macromolecules. Similar to their high-molecular-weight counterparts, these compounds also play pivotal roles in enhancing health, making them attractive candidates for pharmaceutical development [21,22]. These mushroom metabolites align more closely with conventional small-molecule drug development paradigms, owing to their defined chemical structures, improved absorption profiles, and compatibility with established pharmacokinetic and regulatory frameworks [43]. For example, ergothioneine isolated from Pleurotus species exhibits remarkable chemical stability and efficient cellular uptake through the organic cation transporter (OCTN1), resulting in tissue concentrations that are approximately 50–100 times higher than plasma levels [15].

3.2.1. Phenolic Compounds

Phenolic compounds represent one of the most extensively studied classes of mushroom-derived secondary metabolites. Structurally, they are defined by the presence of at least one aromatic ring bearing one or more hydroxyl groups, with molecular complexity ranging from simple phenolic acids to complex flavonoids and tannins [2]. In most edible mushroom species, phenolic acids constitute the dominant phenolic subclass and are commonly grouped into benzoic acid derivatives (C6–C1) and cinnamic acid derivatives (C6–C3). Frequently reported phenolic acids include gallic, caffeic, p-coumaric, protocatechuic, syringic, vanillic, and trans-cinnamic acids, which have been identified across a wide range of edible mushrooms such as Agaricus, Pleurotus, Russula, Lentinus, and Morchella, often in species-specific profiles and concentrations [53,54].
Functionally, mushroom phenolics exert potent antioxidant activity through free-radical scavenging, metal chelation, and inhibition of lipid peroxidation, thereby mitigating oxidative stress associated with chronic diseases. Experimental evidence supports these roles: phenolic-rich extracts of Pleurotus ostreatus significantly improved oxidative balance in 7,12-dimethylbenz(a)anthracene-induced mammary carcinoma models [55], while methanolic and ethyl acetate extracts of C. cibarius and Pleurotus porrigens demonstrated strong radical-scavenging capacity in vitro [56]. Although generally present at lower levels than phenolic acids, flavonoids have also been detected in several mushroom species. Compounds including quercetin, catechin, rutin, myricetin, and kaempferol contribute to the overall antioxidant capacity of mushroom extracts from species such as B. edulis, P. ostreatus, A. bisporus, L. deliciosus, Craterellus cornucopioides, C. cibarius, Calocybe gambosa, and Melanoleuca spp. [57,58].
Recent applications of untargeted metabolomics can also provide deeper insight into the diversity and functional relevance of phenolic compounds in edible mushrooms. High-resolution LC–MS-based profiling enables the simultaneous detection of known phenolic acids (e.g., gallic, caffeic, p-coumaric acids) alongside previously unannotated derivatives that may contribute to antioxidant or anti-inflammatory activity. During fermentation or developmental transitions, metabolomic analyses can reveal shifts in phenylpropanoid-related pathways, allowing correlation of specific phenolic signatures with enhanced radical-scavenging capacity or enzyme-inhibitory effects [59]. Such integrative metabolomic approaches not only expand the catalog of mushroom-derived phenolics but also support their prioritization, standardization, and potential development as small-molecule pharmaceutical candidates.

3.2.2. Terpenoids and Sterols

Terpenoids constitute a structurally diverse group of natural products derived from repeating isoprene units and are classified into mono-, sesqui-, di-, and triterpenes based on their carbon skeletons. In mushrooms, terpenoids, particularly triterpenoids, represent one of the most prominent classes of anti-inflammatory secondary metabolites [60]. Triterpenoids are composed of six isoprene units and typically exhibit complex polycyclic structures, occurring as alcohols, aldehydes, or carboxylic acids. Several triterpenoids isolated from mushrooms have demonstrated notable pharmacological activities. For instance, ganoderic acids C and F from G. lucidum exhibit hypocholesterolemic effects [60], while triterpenoids from Inonotus obliquus suppress inflammation by reducing the production of pro-inflammatory cytokines (TNF-α, IL-1β, IL-6) and mediators such as prostaglandin E2 and NO [61]. Similarly, four triterpenoids isolated from G. lucidum: ganodermanontriol, lucidumol A, ganoderic acid C2, and ganosporeric acid A, exhibited protease inhibitory activity against dengue virus (DENV) at micromolar concentrations comparable to the reference inhibitor 1,8-dihydroxy-4,5-dinitroanthraquinone, underscoring their promising antiviral potential [62]. Antrodia cinnamomea is particularly rich in lanostane-type triterpenoids, including antcin A, B, H, and K, as well as eburicoic and dehydroeburicoic acids, many of which exhibit potent bioactivities [63]. These findings highlight the strong structure–activity relationships governing triterpenoid biofunction.
Recent genomic investigations further illuminate interspecies differences in biosynthetic profiles of these secondary metabolites. Whole-genome sequencing of Trametes sanguinea ZHSJ strain revealed an expanded repertoire of genes encoding terpene synthases and cytochrome P450 enzymes, suggesting substantial, yet underexplored, biosynthetic capacity for structurally diverse terpenoids [64]. Such genomic data provide predictive insight into species-specific metabolite production and offer a strategic framework for prioritizing mushroom taxa with high pharmaceutical development potential.
Sterols, a major subclass of triterpenoids, are characterized by the cyclopentane perhydrophenanthrene nucleus and play essential structural and functional roles in fungal cell membranes [65]. Ergosterol (ergosta-5,7,22-trien-3β-ol) is the predominant sterol in mushrooms and serves as a biochemical precursor to vitamin D2. Beyond its nutritional significance, ergosterol and its derivatives also contribute to therapeutic activities. For example, ergosterol-rich extracts from Auricularia polytricha have demonstrated inhibition of HIV-1 protease activity [66]. Numerous edible mushroom species, including P. ostreatus, P. eryngii, A. bisporus, Russula cyanoxantha, B. edulis, and Coprinus comatus, contain diverse sterol profiles alongside pentacyclic triterpenoids such as oleanolic and ursolic acids, which further contribute to anti-inflammatory and cardioprotective effects [67,68,69,70]. Truffle species (Tuber magnatum, T. melanosporum, T. borchii) further exhibit remarkable sterol diversity, encompassing ergosterol, brassicasterol, campesterol, lanosterol, fungisterol, and dehydroepiandrosterone, emphasizing the chemical and pharmacological richness of fungal sterols [71].

4. From Mycelium to Medicine: Pharmaceutical Development

It is well established that edible mushrooms contain a variety of bioactive compounds with significant therapeutic potential for the development of novel pharmaceutical products. Nevertheless, the quality, safety, and therapeutic efficacy of such products is strongly contingent on the processes involved throughout their development, i.e., from biomass production to the elucidation of bioactive isolates. This section consolidates key information on these procedures, outlining the sequential pathway through which edible mushrooms are transformed into active pharmaceutical ingredients (APIs).

4.1. Sourcing: Origin and Biomass Production

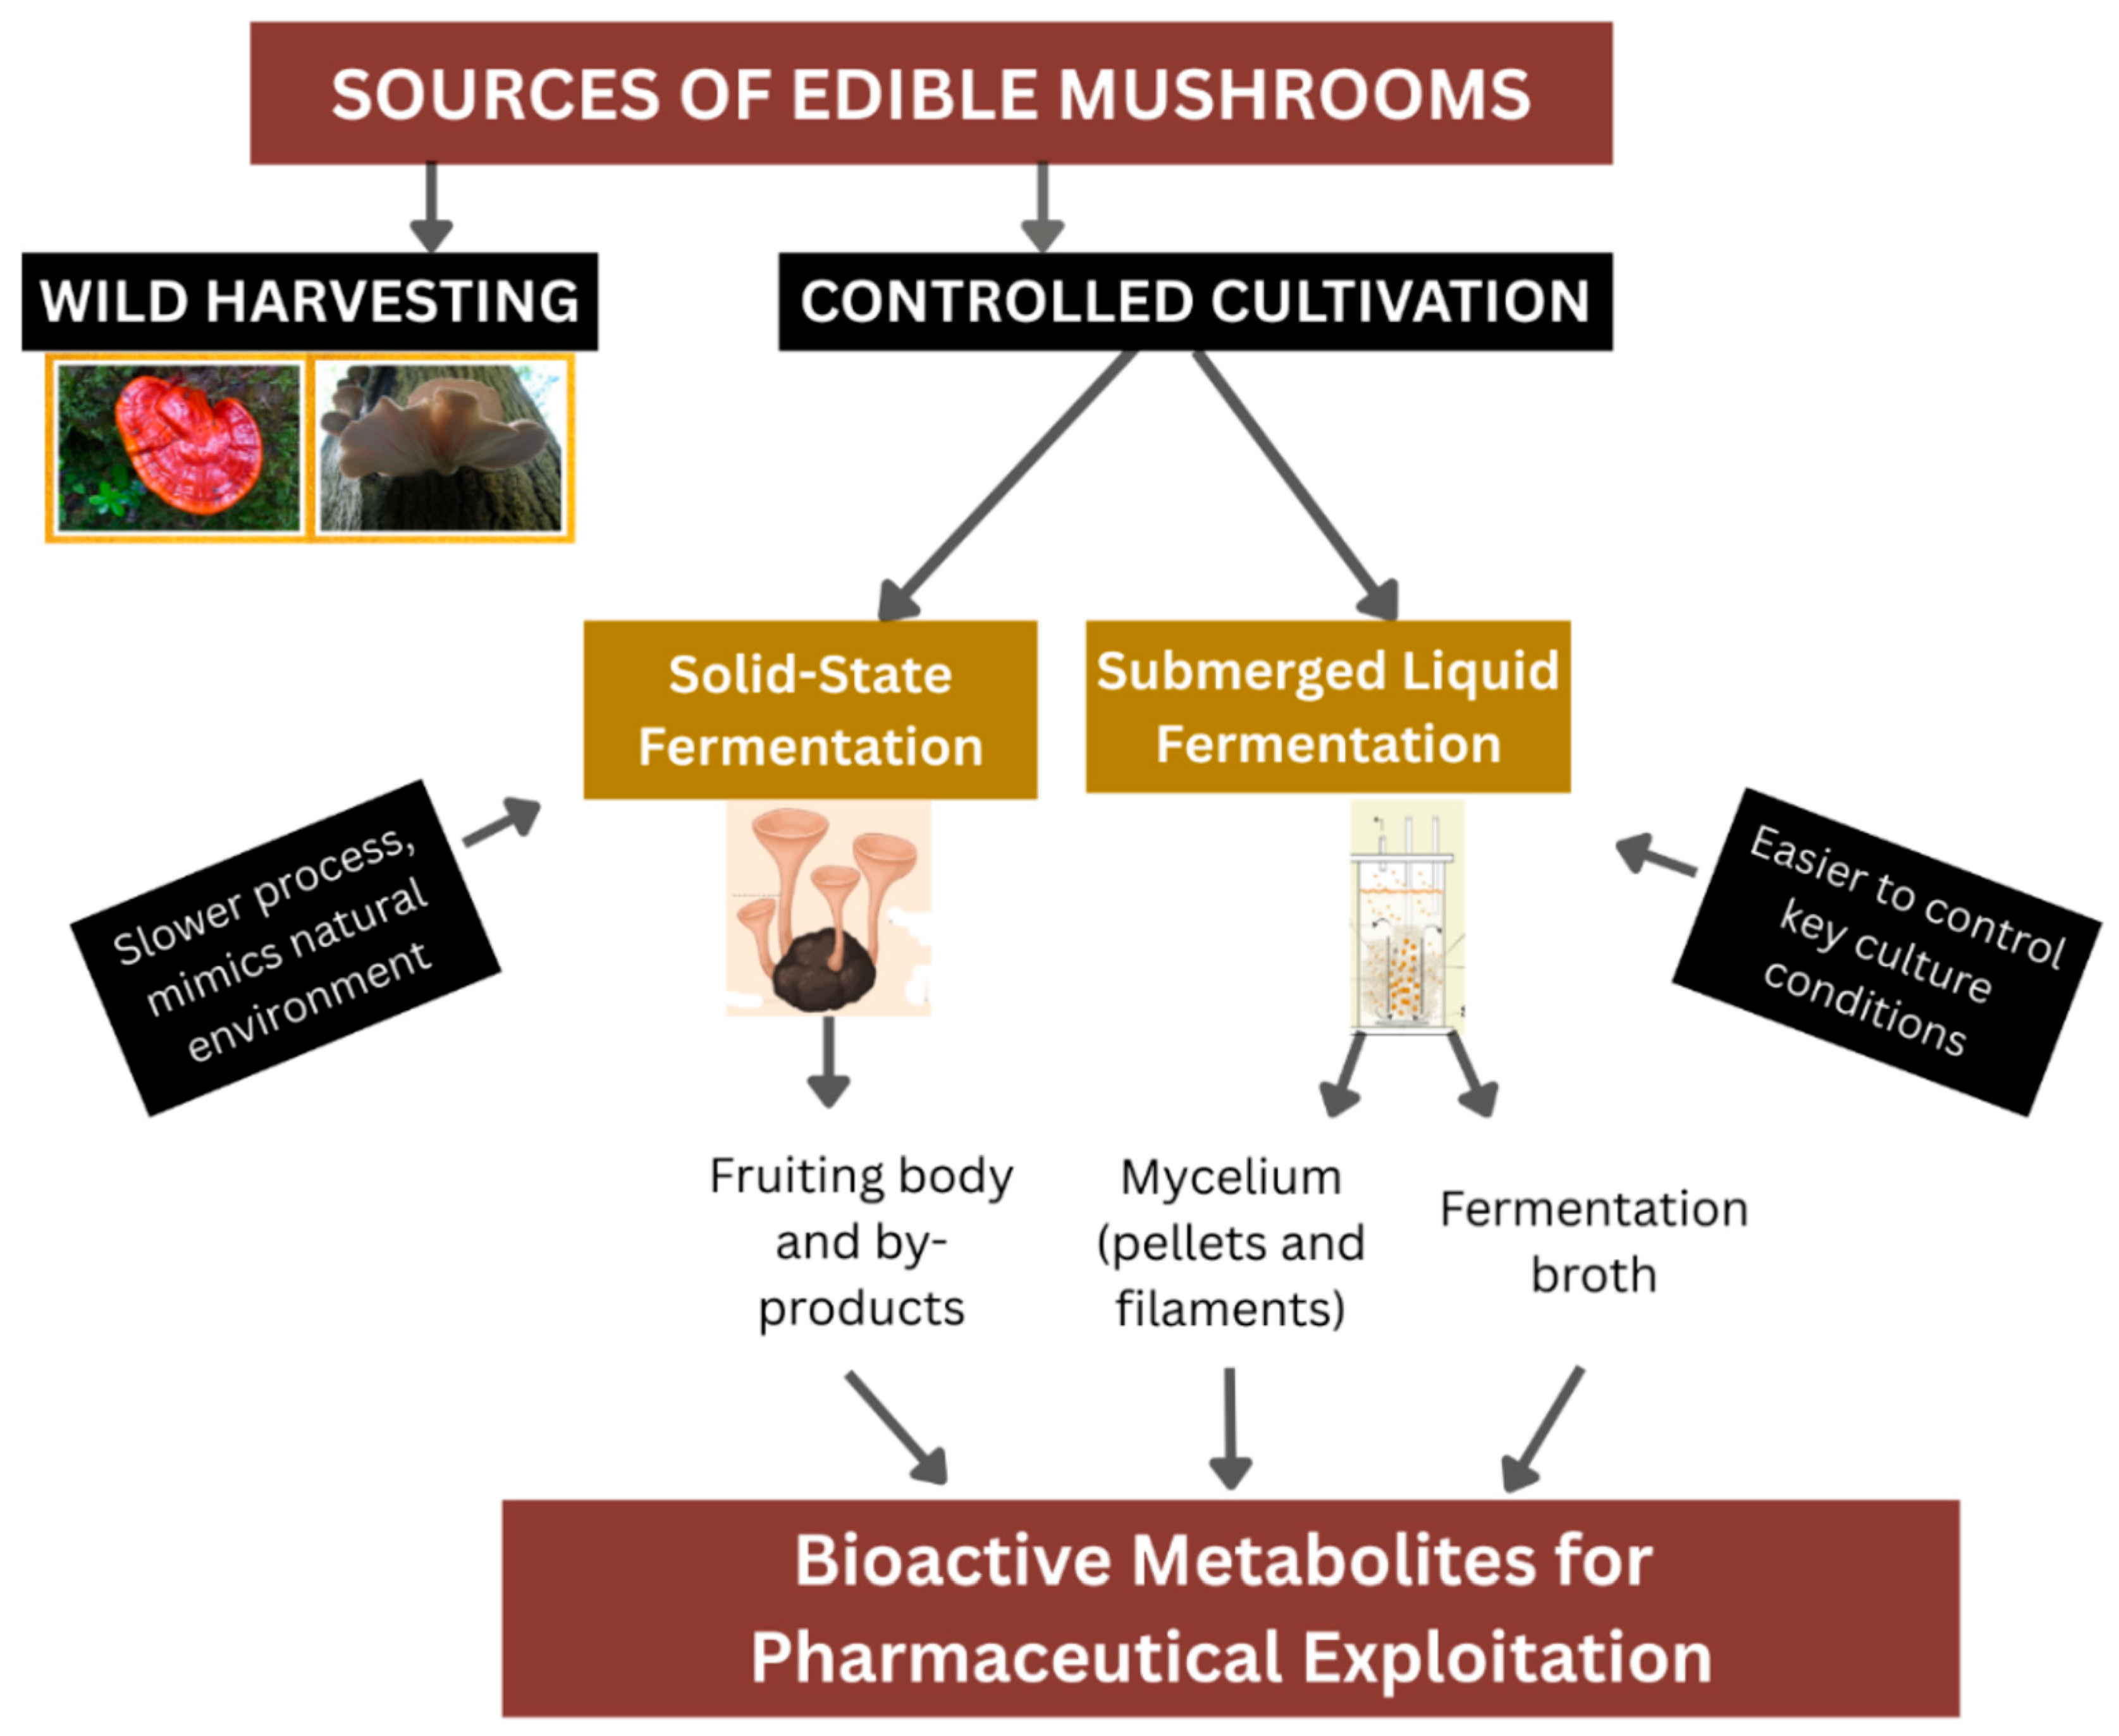
There are presently two possibilities of acquiring edible mushrooms: harvesting from the wild and cultivation (Figure 1). Historically, macrofungal species were sourced exclusively from the wild [2]. However, as their nutritional and therapeutic importance increased, reliance on wild harvesting became unsustainable. Additionally, several factors limit the suitability of wild-sourced mushrooms for pharmaceutical applications, including pest damage, variability in bioactive compound composition, seasonal availability, risk of misidentification with toxic look-alike species, and the potential accumulation of environmental contaminants [72,73,74,75]. Among these concerns, misidentification represents a critical pharmaceutical safety risk, as morphologically similar but toxic mushroom species may be inadvertently harvested and processed, leading to the introduction of toxic compounds into medicinal preparations. Such errors pose serious risks to patient safety and undermine quality control. To overcome these challenges and ensure consistent quality of target bioactive components, controlled cultivation has become essential. Controlled cultivation offers additional advantages, such as rapid biomass production and the ability to generate both fruiting bodies and mycelial biomass under standardized conditions [74]. Mushroom biomass can be produced through solid-state fermentation (SSF) or submerged liquid fermentation (SmF) (Figure 1), both of which aim to produce pure and physiologically active fungal material suitable for downstream pharmaceutical processing [76].

4.1.1. Solid-State Fermentation (SSF)

The production of mushrooms on solid substrate is the most widely applied method for the longest time, owing to its effective utilization of agro-industrial lignocellulosic residues as substrates. This technique supports the conversion of agricultural and industrial waste streams into value-added products, including bioactive compounds relevant to pharmaceutical development (Figure 1) [76]. It remains the most cost-efficient approach for transforming lignocellulosic wastes into a protein-rich edible biomass [2]. For instance, Melanouri et al. [77] demonstrated that ten distinct agro-residues, including wheat straw, poplar sawdust, grape pomace, beech wood shavings, cottonseed cake, corn cobs, coffee residues, olive pulp, barley and oat straw, and rice husk, differentially influenced the cultivation performance of P. ostreatus and P. eryngii. While the magnitude of response varied by substrate type, all residues supported enhanced radial mycelial extension, increased dry biomass accumulation, and elevated extracellular enzyme production, particularly endoglucanase and laccase activities. Similarly, Balenzano et al. [78] reported that grape pomace, used either alone or in combination with wheat straw, effectively supports growth of these mushroom species while improving the nutritional and functional properties of their resulting extracts. This bioconversion process follows a well-defined multistage protocol that includes substrate preparation or composting, inoculation, incubation, fruiting, and harvesting [79]. During the fermentation process, the substrate is incubated under controlled temperature and humidity, enabling mycelial colonization and subsequent fructification over several weeks [76,80]. To prevent biological contamination and resource competition, substrates must undergo high-temperature sterilization prior to inoculation.
Relative to submerged fermentation, SSF offers advantages including lower substrate moisture content and reduced energy requirements [81]. However, a certain level of free water necessary for the optimal development of the mushroom species should be maintained. The low-humidity conditions of the substrate mimic natural fungal habitats, promoting higher fruiting body yields and enhanced concentrations of secondary metabolites important for pharmaceutical applications (Figure 1) [76]. For instance, SSF using the mycelia of P. ostreatus, Hericium erinaceus, and Flammulina velutipes increased the total polyphenol and aglycone isoflavone contents of soybean meal powder by 235.9% and 324.12%, respectively, thereby significantly enhancing its antioxidant activity [81]. Similarly, Nacha et al. [82] reported optimized β-glucan production (54.95% recovery; 79.98% purity) through the SSF of germinated Rice-berry rice with P. ostreatus. Commonly cultivated species using SSF include P. ostreatus and L. edodes [83]. Despite its advantages, the industrial scalability of mushroom production using SSF is constrained by factors such as substrate heterogeneity, species-specific growth variation, heat and mass transfer limitations, pH, and water activity, all of which can influence biomass yield and metabolite profiles [84]. In particular, maintaining the substrate pH within the slightly acidic range (5.0–7.0) optimal for mycelial growth is difficult under SSF conditions, as fungal mycelia continuously secrete organic acids that progressively lower substrate pH during fermentation [84]. This challenge is further exacerbated by the lack of advanced instrumentation for real-time monitoring of internal conditions within solid substrates, especially pH, thereby complicating process control and scale-up [6]. Economically, scale-up requires specialized bioreactor designs and process optimization, increasing production costs and complicating Good Manufacturing Practice (GMP) compliance [8].

4.1.2. Submerged Liquid Fermentation (SmF)

Submerged liquid fermentation (SmF) represents a promising alternative strategy for the controlled production of high-value mycelial biomass and bioactive metabolites from edible mushrooms. This cultivation approach has attracted considerable attention due to its efficiency, scalability, and suitability for producing compounds with broad applications in the nutraceutical and pharmaceutical industries [76,84]. Although SSF remains the predominant method for mushroom cultivation, advances in submerged fermentation technologies continue to improve the feasibility of generating uniform, reproducible, and high-quality mushroom biomass under controlled conditions [85]. The production of nutritionally and therapeutically valuable mushroom biomass via SmF typically involves a series of biotechnological steps that encompasses the preparation of nutrient-rich liquid culture medium, regulation of physicochemical parameters and separation of the resulting mycelial biomass (often in the form of pellets or filamentous structures) from the fermentation broth [76,86].
Unlike solid-state production, SmF offers several advantages, including shorter fermentation cycles (typically 3–7 days), reduced contamination risks, and precise control over cultivation conditions that influence biomass accumulation and metabolite synthesis, such as temperature, pH, and dissolved oxygen levels [6]. For example, Krasnopolskaya et al. [87] demonstrated that F. velutipes exhibited maximal ACE production at 20 °C, whereas optimal biomass accumulation occurred at 30 °C. The influence of such physicochemical factors on mushroom growth and metabolite production in SmF systems has been comprehensively described by Perveen et al. [88].
An additional advantage of SmF lies in the ease of recovering extracellular metabolites, such as bioactive exopolysaccharides, secreted directly into the fermentation broth. Nevertheless, the choice between SSF and SmF ultimately depends on productivity, metabolite yield, and biological efficacy. For instance, laccases produced by P. ostreatus strain ATCC 32783 under SmF and SSF conditions exhibited distinct isoenzyme profiles and levels of enzymatic activity [89]. Bioactive compounds sourced from mycelia produced using SmF tend to exhibit greater compositional consistency, as fermentation parameters can be finely optimized to enhance metabolite quality and bioactivity [76]. Papaspyridi et al. [90] demonstrated the considerable potential of submerged liquid fermentation in batch-operated stirred-tank bioreactors for producing P. ostreatus mycelial biomass with an enhanced metabolic profile. Using this approach, the authors confirmed the biosynthesis of trans-3,4-dihydro-3,4,8-trihydroxynaphthalen-1(2H)-one, indole-3-carboxylic acid, 3-formylpyrrole, and 4-hydroxybenzoic acid—compounds identified as novel metabolites of pharmaceutical relevance. Similarly, SmF has been employed for the cultivation of S. commune, Lentinus polychrous, L. edodes, G. lucidum, and Lentinus squarrosulus, yielding extracts that exhibited significant antioxidant activity, thereby highlighting their potential for further development into pharmaceutical products [91].
For pharmaceutical applications, scaling up SmF processes in bioreactor systems such as bubble columns, stirred tanks, and airlift bioreactors is essential to ensure industrial feasibility. This requires the optimization of bioprocess efficiency and reactor design such that pilot-scale and industrial-scale fermentations achieve yields comparable to or exceeding those obtained at laboratory scale [6,88]. Accordingly, advances in bioreactor engineering and process control are therefore critical for translating submerged mushroom cultivation into large-scale pharmaceutical production platforms. However, high operational costs associated with aeration, agitation, and energy input may limit economic feasibility on the industrial scale. In addition, maintaining genetic stability and ensuring reproducible secondary metabolite production over prolonged fermentation cycles remain key industrial challenges [88].

4.2. Pre-Extraction Processing: Preservation and Disruption

Following the harvest of fruiting bodies or the recovery of cultivated mycelial biomass, immediate preservation is essential to maintain post-harvest quality. Edible mushrooms are highly perishable, with a short shelf life of approximately 1–3 days, and are prone to rapid deterioration due to both intrinsic metabolic activity and extrinsic environmental factors [92,93]. For edible mushrooms intended for pharmaceutical applications, stabilization of the biomass through drying is a critical downstream process, as it prevents degradation and preserves the integrity of bioactive constituents.
A range of drying techniques is employed in mushroom processing, including natural air drying, hot-air drying, freeze-drying, microwave drying, vacuum drying, solar drying, and infrared radiation drying. Each method exerts distinct effects on the chemical composition and stability of mushroom bioactives [8,94]. For instance, Gąsecka et al. [95] reported significant reductions in polysaccharide content in Leccinum scabrum and H. erinaceus following hot-air drying, attributable to the thermal degradation of heat-sensitive polysaccharides into oligosaccharides. Similarly, Wei et al. [96] observed notable differences in polysaccharide extraction yields from Cordyceps militaris depending on the drying method used, with infrared drying (3.61%) outperforming freeze-drying (2.60%) and hot-air drying (2.19%). These findings underscore the importance of selecting an appropriate drying technique during the development of mushroom-based pharmaceutical products. Among available methods, freeze-drying or lyophilization is often preferred by pharmaceutical industries because the low temperatures employed minimize thermal degradation and allow for superior retention of bioactive compounds comparable to those in fresh mushroom material [94].
Beyond preservation, effective disruption of the mushroom cellular structure is necessary to facilitate the extraction of intracellular bioactive compounds. Mushroom cells are protected by a robust chitin-rich cell wall that limits solvent penetration. To overcome this barrier, dried mushroom biomass is typically subjected to mechanical size reduction using mills or homogenizers to produce small fragments or fine powders [97]. Grinding aims to achieve an optimal particle size that enhances solubility and improves extraction efficiency [94]. Extraction yields are strongly influenced by particle size, as finer particles provide increased surface area and greater solvent–matrix interaction [8]. For example, Xiaokang et al. [98] reported that reducing the particle size of L. edodes from 4.75 to 1.75 mm resulted in a corresponding increase in total phenolic content, rising from 4.90 to 6.35 mg GAE/g.
Collectively, drying and grinding represent critical pre-extraction steps that directly influence the stability, accessibility, and recoverability of mushroom-derived bioactive compounds. Their careful optimization is therefore crucial for the successful pharmaceutical application of edible mushroom extracts.

4.3. Extraction: Liberating Compounds from the Fungal Matrix

Extraction constitutes the primary step in isolating pharmaceutical-relevant bioactive compounds from raw mushroom biomass. At its core, the extraction process involves several sequential events: penetration of the solvent into the solid mushroom matrix, dissolution of soluble components, diffusion of the solutes out of the solid phase, and subsequent recovery of the extracted compounds [8,99]. The efficiency of extraction is primarily determined by the dissolution and diffusion dynamics of these steps and is influenced by factors such as the physicochemical properties of the extraction solvent, particle size of the raw material, solvent-to-solid ratio, extraction temperature, and extraction duration [8]. The choice of extraction solvent is a critical determinant of process efficiency and is governed by factors such as solubility, selectivity, safety, and cost. In accordance with the principle of “like dissolves like,” optimal extraction is achieved when the polarity of the solvent closely matches that of the target solutes [99].
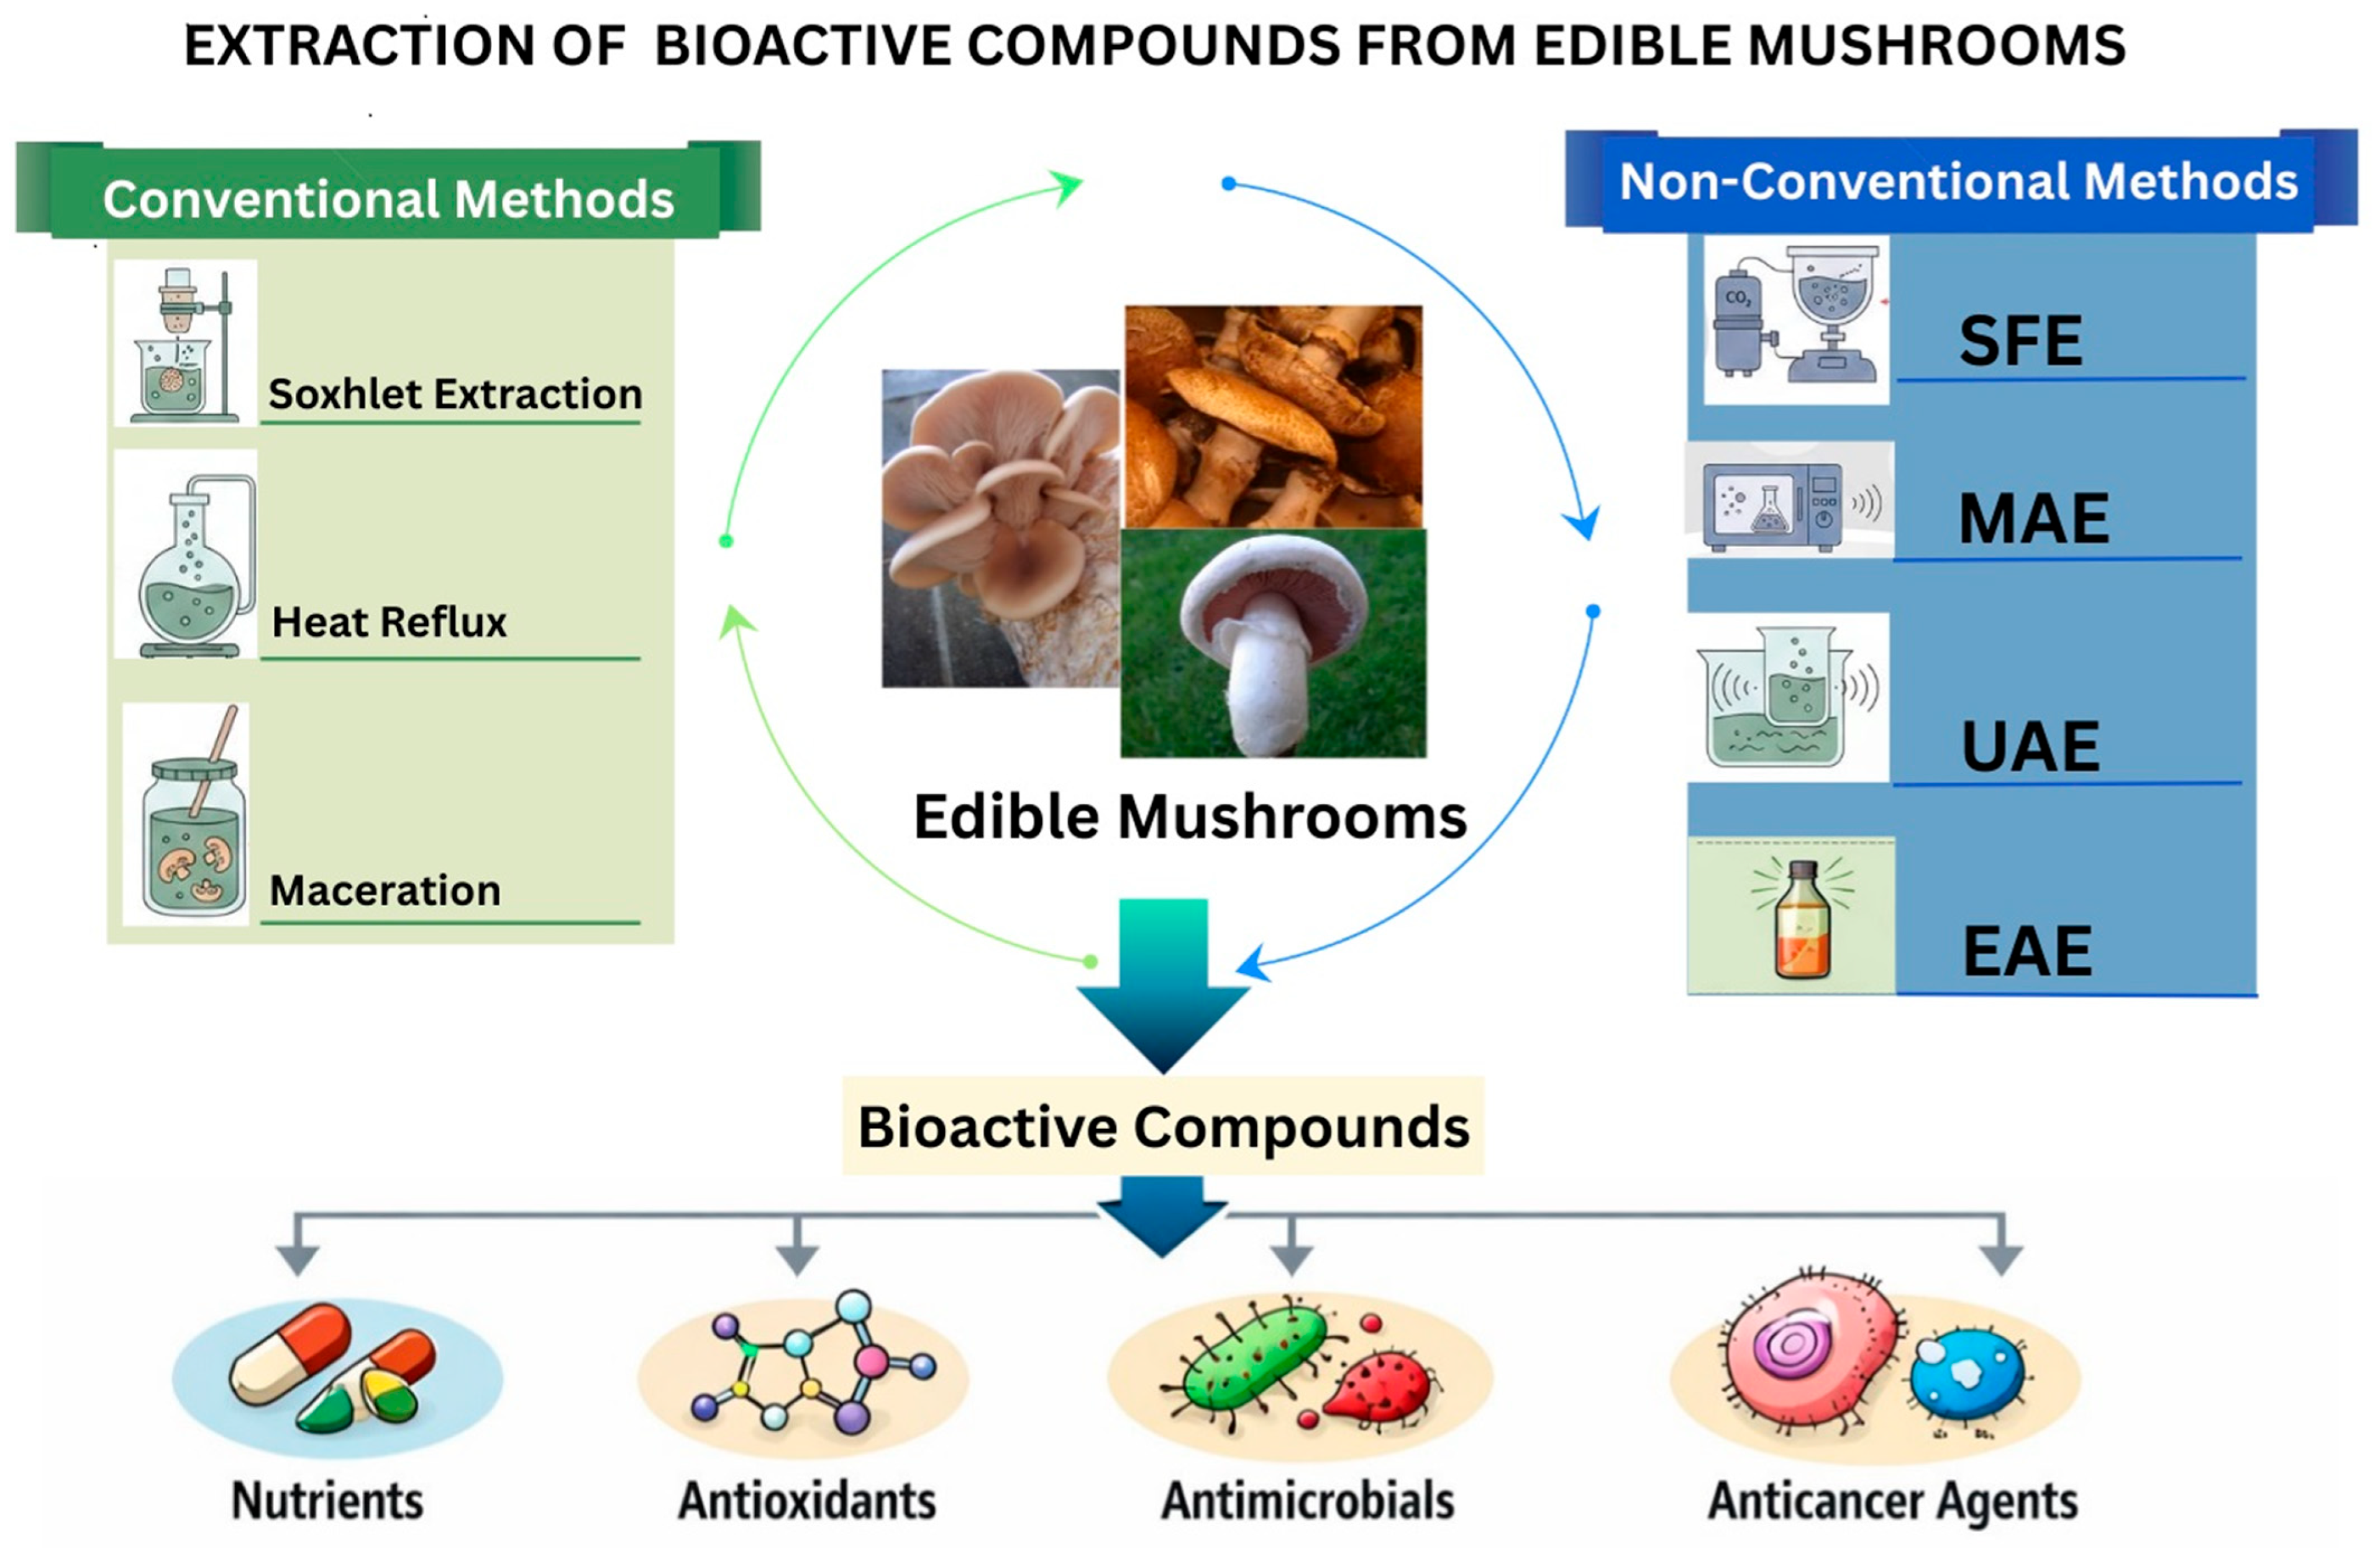
A wide range of conventional and advanced extraction technologies is currently employed for mushroom bioactives (Figure 2). Limitations associated with conventional techniques, such as high solvent consumption, long extraction times, and energy inefficiency (Table 1), have driven the increasing adoption of advanced extraction technologies. A comparative overview of these methods, including their respective advantages and drawbacks, is presented in Table 1. The selection of an appropriate extraction method must account for the chemical nature of the target compounds, the complexity of the fungal matrix, desired yield, and environmental sustainability [100]. As summarized in Table 1, this choice involves balancing extraction efficiency and selectivity against processing time, solvent and energy demands, and the potential degradation of thermolabile compounds, with advanced techniques generally providing higher yields and improved process control compared to conventional solvent-based methods.

4.3.1. Conventional Solvent-Based Methods

Conventional extraction of mushroom bioactive compounds is predominantly based on solid–liquid extraction using water or organic solvents (majorly methanol and ethanol). Among these approaches, hot-water extraction is widely employed, particularly for polar compounds such as water-soluble polysaccharides. This method is valued for its simplicity, cost-effectiveness, safety, and environmental compatibility [18]. However, the elevated temperatures and prolonged extraction times commonly required (Table 1) increase the risk of degrading thermolabile bioactive constituents [3,101]. Sequential extraction strategies, typically involving water followed by alcohol, have also been applied to recover high-value mushroom-derived compounds [101]. Despite improved extraction breadth, this approach often entails the use of high concentrations of organic solvents (30–98.6%) and extended extraction durations ranging from 1 to 24 h, which may limit its industrial and environmental viability (Table 1) [3].
For compounds of moderate to low polarity, such as lipids and certain polyphenols, conventional techniques including Soxhlet extraction and maceration (Figure 2) are commonly employed. In Soxhlet extraction, the solvent is heated to reflux, evaporated, and subsequently condensed onto the mushroom material contained within a cartridge. Continuous percolation of the solvent through the solid matrix enables the solubilization and transfer of target compounds to a collection flask via a siphoning mechanism [13]. In contrast, maceration involves soaking ground mushroom material in organic solvents at ambient temperature, allowing gradual softening of the matrix and diffusion of bioactive constituents into the solvent. Periodic agitation may be applied to enhance extraction efficiency [102]. Table 2 summarizes information on recent studies employing conventional solvent-based methods for the extraction of mushroom bioactives. The collative evidence in Table 2 indicates that conventional solvent-based extraction efficiency in mushrooms is strongly influenced by solvent polarity, temperature, and extraction duration, with aqueous and hydro-alcoholic solvents generally favoring polysaccharide and phenolic recovery, while non-polar solvents such as hexane and diethyl ether preferentially extract lipophilic compounds, albeit often at lower yields.

4.3.2. Advanced/Green Extraction Techniques

A range of advanced and environmentally benign extraction technologies has been developed for the recovery of pharmaceutical-relevant bioactive compounds from biological resources, including edible mushrooms (Figure 2). These approaches are attracting increasing interest within the pharmaceutical industry because they enable more sustainable processing, shorten extraction time, and often improve extraction efficiency and product quality compared with conventional methods (Table 1).
Enzyme-Assisted Extraction (EAE)
Enzyme-assisted extraction (EAE) exploits the catalytic activity of specific enzymes to degrade structural components of the mushroom cell wall and membranes, thereby facilitating the release of intracellular and bound bioactive compounds. The fungal cell wall is primarily composed of chitin (β-1,4-N-acetylglucosamine) and glucans (β-1,3 and β-1,6 linkages), which can be selectively hydrolyzed using enzymes such as chitinases and glucanases, leading to enhanced extraction efficiency [12,101]. For example, Enman et al. [127] reported the extraction of eritadenine, a hypocholesterolemic compound, from L. edodes using a mixture of α- and β-glucanases. Although the enzymatic pretreatment only marginally increased the yield during subsequent methanolic extraction, it demonstrated the feasibility of enzyme-mediated release of target metabolites. Beyond glycosyl hydrolases, enzymes such as cellulases, pectinases, and proteases are also commonly employed in EAE protocols [99]. Nguyen and Nguyen [128], for instance, obtained a crude extract rich in amino acids, flavonoids, phenolics, proteins, reducing sugars, sucrose, and β-glucans from Pleurotus sajor-caju following pretreatment with exogenous cellulase at 50 °C and pH 5.5 for 8 h.
From an industrial perspective, EAE is particularly attractive because it operates under relatively mild conditions, which helps preserve the structural integrity and bioactivity of thermolabile compounds [129]. Compared with conventional methods, EAE generally requires lower temperatures and shorter processing times while delivering higher extraction yields (Table 3). Zhu et al. [130] demonstrated a 67.72% increase in polysaccharide yield from H. erinaceus using a cellulase:pectinase:trypsin mixture (2:2:1) under optimized conditions (pH 5.71, 52.03 °C, 33.79 min) relative to hot-water extraction. Similarly, Hwang et al. [123] showed that enzymatic extraction using Viscozyme L (a multi-enzymatic complex containing a wide range of carbohydrases) at pH 4.5 and 50 °C for 2 h produced higher levels of β-glucans, triterpenoids, gallic acid, and caffeic acid from I. obliquus than conventional hot-water extraction at 100 °C.
Despite these advantages, EAE presents several practical limitations. The process typically involves multiple downstream steps, including cell lysis, filtration, and centrifugation, which increase technical complexity. In addition, careful optimization and storage conditions are required to maintain enzyme stability and activity [12]. The relatively high cost of commercial enzymes also remains a major constraint for large-scale industrial application of EAE.
Ultrasonic-Assisted Extraction (UAE)
Ultrasonic-assisted extraction (UAE), commonly referred to as sonication, is another emerging green technique for the recovery of bioactive compounds from edible mushrooms. Its effectiveness has been demonstrated in several studies (Table 3); for example, Quintero-Cabello et al. [131] successfully extracted ergosterol, a compound with hypocholesterolemic properties, from Neolentinus lepideus using ultrasound treatment. The underlying mechanism of UAE is acoustic cavitation, which occurs when ultrasonic waves propagate through the solvent medium. These waves are generated by a transducer integrated into either an ultrasonic probe or bath system, converting electrical energy into mechanical vibrations [132]. Cavitation involves the formation, growth, and subsequent implosive collapse of microbubbles, producing localized high shear forces and micro-turbulence. This phenomenon disrupts the mushroom cell wall, enhances solvent penetration, and hastens mass transfer between the solvent and the solid matrix [13,92,133].
As a result, UAE significantly reduces extraction time by promoting faster dissolution and diffusion of solutes. The enhanced heat and mass transfer also allows for an extraction to be performed at relatively lower bulk temperatures, thereby minimizing the degradation of thermolabile compounds while improving overall extraction yield [99,101]. For instance, Hwang et al. [123] reported higher triterpenoid yields from I. obliquus using ultrasound extraction (139 W, 42 kHz, 50 °C) in relation to conventional hot-water extraction (100 °C). Similarly, Cheung et al. [134] observed increased polysaccharide yields from Cordyceps sinensis Cs-HK1 with rising ultrasound intensity (2.44 to 44.1 W/cm2), with UAE outperforming water extraction over treatment times of 10–80 min. Furthermore, ultrasound treatment significantly increased the recovery of polysaccharides from dried and milled A. bisporus by-products relative to untreated samples, with a maximum extraction yield of 4.7% obtained after 15 min at an amplitude of 100 μm [135].
Efficient application of UAE requires careful optimization of processing parameters, including ultrasonic power, extraction time, solvent-to-solid ratio, and temperature. Ma et al. [136] identified optimal conditions for extracting polysaccharides from black fungus mushroom as 350 W ultrasonic power, a fivefold solvent volume, 35 min extraction time, and 90 °C. Likewise, Gogoi et al. [132] demonstrated that ultrasound treatment time, temperature, and solid-to-solvent ratio significantly influenced the recovery of phenolic acids from Pleurotus citrinopileatus, with distinct optimal conditions for aqueous (44 °C, 14 min, and 20 mL/g) and ethanolic (39 °C, 13 min, and 20 mL/g) extracts. From an industrial perspective, ultrasonic probe systems are generally preferred over bath systems because they deliver higher energy density through a localized tip surface, resulting in more efficient cavitation and improved extraction performance [135].
Microwave-Assisted Extraction (MAE)
Microwave-assisted extraction (MAE) is based on the rapid heating of moisture within mushroom tissues, which generates internal pressure sufficient to disrupt cellular structures and promote the release of intracellular bioactive compounds [3]. This process is enabled by the dielectric properties of mushrooms, whereby microwave energy interacts with polar molecules through ionic conduction and dipole rotation, resulting in volumetric heating of the solid matrix [99]. Microwaves are electromagnetic waves composed of oscillating electric and magnetic fields operating within a frequency range of 300 MHz to 300 GHz, with 915, 2450, 5800, and 22,125 MHz being the most commonly applied frequencies in industrial and laboratory-scale heating [3,98,101].
Unlike conventional extraction, where heat is transferred from the external source to the medium via conduction and convection, MAE generates heat directly within the irradiated material. This selective internal heating minimizes energy loss to the surroundings and accelerates mass transfer, thereby enhancing extraction efficiency [101]. Consequently, MAE is recognized for its ability to achieve high extraction yields within short processing times (Table 3) while reducing solvent consumption and overall energy input.
Several studies have demonstrated the effectiveness of MAE for extracting mushroom bioactives (Table 3). Using response surface methodology, Maeng et al. [110] optimized the MAE of total phenolics from T. versicolor, achieving a maximum yield of 470 mg GAE/100 g in 3.8 min with 40% ethanol and a microwave power of 125 W, which exceeded yields obtained by reflux extraction (434 mg GAE/100 g). Similarly, Özyürek et al. [137] successfully extracted polyphenols from Terfezia boudieri, B. edulis, and Lactarius volemus under optimized MAE conditions using methanol–water (80:20, v/v) at 80 °C for 5 min. Comparative studies by Xiaokang et al. [98] further showed that MAE (solid-to-liquid ratio 1:40, 600 W, 15 min) produced significantly higher phenolic contents (11.23 mg GAE/g) from L. edodes than organic solvent-based extraction (3.68 mg GAE/g). In addition, Zhang et al. [138] reported enhanced recovery of gallic acid, protocatechuic acid, catechin, syringic acid, myricetin, and quercetin from Agaricus blazei using MAE (60% ethanol, solvent-to-solid ratio 1:30, 110 °C, 500 W, 5 min) compared with heat reflux extraction and maceration. Despite these advantages, the widespread industrial application of MAE remains constrained by high equipment and operational costs, which currently limit its scalability.
Supercritical Fluid Extraction (SFE)
Supercritical fluid extraction (SFE) is particularly gaining increasing interest from the food and pharmaceutical industries due to its high extraction efficiency and environmentally benign characteristics. In SFE, the extraction medium is a supercritical fluid, defined as a substance maintained above its critical temperature and pressure, where distinct liquid and gaseous phases no longer exist. Under these conditions, the fluid exhibits intermediate physicochemical properties, combining liquid-like solvation capacity with gas-like diffusivity, which enhances mass transfer and penetration into solid matrices [8,13].
Table 3. Application of advanced and non-conventional extraction techniques for the recovery of bioactive compounds from edible mushrooms.
Mushroom Material (Pre-Treatment)Extraction TechniqueExtraction Solvent/MediumOperating ConditionsOptimized Extraction ParametersTarget Bioactive Compound(s)Extraction Yield/Recovery EfficiencyReference
L. edodes—powdered into 850 μm particle size with an electric millUAE combined with autoclavingWaterP = 550 W, A = 60%, t = 60 min, Solvent/solid ratio = 1:30 (w/v), f = 20 kHzNAPolysaccharides16.3% yield, which was significantly higher than the yield of hot water extract[139]
Pleurotus citrinopileatus—tray dried and powdered using a household grinderUAEWater and EthanolUltrasonic bath, T = 30–55 °C, t = 8–20 min, solvent/solid ratio = 20–50 mL/g, P = 200 W, f = 40 kHzWater extract
= 44 °C, 14 min, and 20 mL/g
Ethanol extract = 39 °C, 13 min, and 20 mL/g
Total phenolics and flavonoidsUltrasonication treatment time, temperature and solid to solvent ratio
influenced the yield of phenolic acids
[132]
Flammulina velutipes—freeze-dried and powdered via superfine comminution technique (300 mesh)UAEWaterUltrasonic probe horn of 10 mm diameter, solvent/solid ratio = 1:25 w/v, P = 620 W, T = 45 °C, t = 20 min, f = 20 kHzNAPolysaccharides (FVP)UAE resulted in higher yield (5.59%) of FVP content compared to hot-water extraction (4.45%)[140]
Armillaria mellea—oven dried, crushed and sieved through a 60 mesh sieveUAEWaterUltrasonic bath, T = 70 °C, P = 280 W, t = 40 min, solvent/solid ratio = 1:20 g/mLNAPolysaccharides (AMPs)3.86% yield[141]
EAENA2.3% of cellulase: papain (1:1), material-liquid ratio = 1:20 g/mL, pH = 5, T = 40 °C, t = 140 min5.21% yield
P. eryngii—dried and powderedUAEWater P = 464 W, f = 80 kHz, T = 60 °C, t = 3.5 h, solid–liquid ratio = 1:36 g/mLNAPolysaccharide (PEP) 4.4% yield of crude PEP with a
carbohydrate content of 44.4%
[142]
Suillus bovinus—lyophilized and ground by an electric grinderUAE93.6% MethanolSolvent/solid ratio = 1.3% (w/v), f = 20 Hz, P = 70 W, T = 60 °C, t = 5 min, A = 16.86%, 0.71 s−1 cyclesNATotal phenolicsUAE is an effective method for the recovery of phenolic compounds from wild and cultivated edible mushrooms[143]
A. auricula-judae—freeze-dried and ground (80-mesh)UAEWater, methanolSolvent-to-sample ratios = 10:1, 20:1, 30:1 mL/g; pulse duty cycles = 0.2, 0.6, 1.0 s−1; T = 10, 40, 70 °C; t = 10 min1:18 g/mL methanol, T = 59 °C and pulse duty cycle of 0.7 s-1.Total phenolicsA recovery rate of 94.85% for TPC was achieved using this method[144]
A. bisporus—air-dried and ground using a blenderMAEEthanol/water (80:20, v/v)Ethanol concentration = 10–90%, t = 1–30 min, solvent/solid ratio = 5–20 mL/0.2 gt = 16 min; solvent/solid ratio = 12.9 mL/0.2 g; ethanol concentration = 58%Total phenolics14.82 mg GAE/g[145]
P. ostreatus and P. eryngii—air dried and groundMAEWater, absolute ethanol, and ethyl acetateSolid-to-solvent ratio = 1:30 (w/v), T = 80 °C, t = 5 min, P = 30 to 100 W depending on the solventNATotal phenolicsThe ethyl acetate extracts of both mushroom species were most biologically effective[78]
Schizophyllum commune—powderedMAEWaterSolvent/solid ratio = 1:4 (w/w); T = 80 °C, 100 °C, and 120 °C; t = 2, 6, and 10 minT = 80 °C, t = 2 min, solvent/solid ratio = 1:4 (w/w)Multiple compounds, including amino acids16.76% to 34.18% crude extract yield (wet basis)[146]
Multiple Pleurotus spp.—freeze-dried and powderedMAEMethanol and water0–30% methanol in water, solvent/sample ratio = 10:1–20:1 mL/g, T = 40–70 °C, P = 800 W, t = 10 minPure water as a solvent, solvent/sample ratio = 17.5:1, T = 44 °C, t = 10 minPhenolic compounds: p-coumaric acid, t-cinnamic acid, p-hydroxybenzaldehyde, p-hydroxybenzoic acid, quercetin-3-glucoside, gallic acid, and vanillic acidThe developed UAE method demonstrated high accuracy (>85% recovery) and precision (CV < 10%), confirming its reliability for the profiling of phenolic compounds in oyster mushrooms[147]
D. indusiata—air dried and pulverizedMAEWaterSolid/liquid ratio = 1:40, t = 7 min, P = 150 WNAPolysaccharidesUAE had a higher yield than MAE; however, the sequential combination of both techniques produced higher yields than both individually[125]
UAESolid/liquid ratio = 1:40, P = 600 W, T = 80 °C, t = 25 min
L. edodes—dried mushroom bodies were pulverized into a powder using an electric millUAENAUltrasonic probe horn (3 mm-diameter), f = 20 kHz, P = 750 W, A = 60% (0.87 W/mL), t = 40 minOptimized sequential extraction (EAE followed by UAE): enzyme 0.28% (w/v), A = 62%, and (NH4)2SO4 saturation 69%Proteins6.9% yield[148]
EAE0.3% of cellulase (50 U/mg), T = 45 °C, t = 1 h, pH 4.54.9% yield
A. bisporus (white strain and brown strain), L. edodes, P. ostreatus (HK35 and Spoppo)—air dried and ground by means of a cross beater millUAEAlkaline mediumLaboratory scale: Ultrasonic probe, P = 400 W, f = 20 kHz, 30 g of sample mixed with 0.1 mol/L NaOH, T ≤ 45 °C
Medium scale: P = 1000 W, f = 24 kHz, increase in mass of feedstock and volume of solvent by 10 times
NAProteins7–17% yield[149]
EAE10 mM phosphate buffer Protease (2.59 AU/G) or papain (1.5 units/mg); enzyme to substrate ratio = 1% (w/w); t = 2 h; protease pH 6.5–8.5 at T = 60 °C; papain pH 6.0–7.0 at T = 65 °C23–24% yield
A. bisporus—hot air oven dried and ground into fine powder (80 mesh)EAEWater12.36 μL of α-amylase (3000 U/g) and 168 μL of amyloglucosidase (3300 U/g), pH 4.5, T = 50–55 °C, t = 4 h, solvent/solid ratio = 3:25 g/mLNAPhenolic acids, flavonoids, and total glucans26.48–31.30% yield[150]
L. saccatum, P. ostreatus, C. cornucopioides, R. cyanoxantha and C. cibarius—airdried and ground in a blender into 0.132 mm, 0.277 mm, 0.433 mm, 0.294 mm and 0.347 mm, respectivelySFESc-CO2 (purity 99.9% v/v)T = 40 °C, p = 30 MPa, CO2 flow rate of 1.94 kg/h, t = 0.5–4 ht = 4 hLipids0.807–3.316% yield[108]
A. bisporus—lyophilised and powderedSFECO2 (>99.998% purity) and ethanol (solvent modifier)Flow rate of 4 mL/min (including carbon dioxide and co-solvent), p = 70–300 barp = 244 bar, T = 56 °C, 8% (v/v) co-solventErgosterol6.23 mg/g d.w[151]
P. ostreatus—fresh material ground in a blenderSFECO2 and water as co-solventT = 393.15–433.15 K, p = 15–35 MPa, 10 to 20% H2O, CO2 flow rate of 2.5 L/min−1p = 25 MPa, T = 433.15 K, 20% H2OPolysaccharides2.06–30.73% yield[105]
Cordyceps sinensis—powder of average particle size 300 μmSFESc-CO2 and ethanol 1% (v/v) as co-solventp = 200, 250, 300 and 350 bar; T = 40, 50 and 60 °C; CO2 flow rate of 0.4 L/h, t = 1.5–2 hT = 60 °C, p = 300 bar, t = 2 hCordycepin and flavonoids0.53–0.75% (w/w)[152]
Pleurotus pulmonarius—freeze-dried and ground to a fine powder of pore size 0.12 mmSFESc-CO2 with and without 5% ethanol as co-solventp = 38 MPa, T = 80 °C, t = 2.7 hNAFatty acids, total phenols and ergosterol0.36% (without co-solvent)–0.93% (with co-solvent) yield[153]
UAEWaterUltrasound bath, t = 1 h, T = 37 °C45.14–63.32% yield
Tuber aestivum and Terfezia claveryi—lyophilized and powdered (< 0.5 mm)PLEWater, ethanol (100%) and water:ethanol (1:1 v/v)Accelerated Solvent Extractor; T = 50, 115, and 180 °C; t = 5, 17.5, and 30 minp = 16.7 MPa, T = 180 °C, t = 30 minMultiple compounds, including β-glucans and sterolsVaried by species and solvents used[154]
P. ostreatus (powdered) and G. lucidum (fine pieces)—both lyophilizedPLE (ASE)WaterT = 50–180 °C, t = 5–30 min, p = 10.2–11.7 MPaT = 180 °C, t = 26 min for P. ostreatus; and T = 180 °C, t = 22 min for G. lucidumPolysaccharides (β-d-glucans)11.9% (G. lucidum); 30.3% (P. ostreatus) (w/w) [155]
L. edodes—oven dried and ground into fine particles (500 μm) using a blenderPLE (ASE)Water, ethanol (60% v/v)T = 40–160 °C, t = 5–30 min, p = 10.3 MPaT = 142 °C, t = 5 minEritadenine652 mg/100 g d.w[156]
P. eryngii, H. erinaceus and P. citrinopileatus—dried and powdered using a Moulinex grinderPLE (SWE)WaterLiquid to solid ratio = 12 (w/w), T = 160 and 190 °CT = 190 °CTotal glucans11.63–47.57% yield, depending on species and temperature[157]
Agaricus blazei fruiting bodyPLE (SWE)WaterT = 120, 140, 160, or 200 °C; p = 2 and 5 MPa; t = 5–240 minNAPolysaccharide (FIII-2-b)Subcritical water extracts from the fruiting body or mycelium of A. blazei significantly inhibited the expression of immune checkpoint molecules and Axl[158]
A. blazei mycelium—air driedT = 160 °C, t = 5 min
NA—not reported in the cited study; t = time; P = power; p = pressure; T = temperature; f = frequency; A = amplitude; GAE—gallic acid equivalent.
Among supercritical fluids, carbon dioxide (SC-CO2) is the most widely used solvent owing to its favorable attributes, including a low critical temperature (31 °C), tunable selectivity, low cost, non-toxicity, high density, low viscosity, and high diffusivity [99,133]. Moreover, the U.S. Food and Drug Administration has designated SC-CO2 as a “Generally Recognized as Safe” (GRAS) solvent, making it particularly suitable for pharmaceutical and food-related applications.
The solvating power of SC-CO2 can be precisely modulated by small variations in pressure and temperature near the critical point. Although its inherently low polarity favors the extraction of non-polar compounds such as lipids and sterols, the addition of polar co-solvents (modifiers), such as ethanol, can substantially expand its extraction range to include moderately polar bioactive compounds [101]. For example, Mishra et al. [152] employed 1% (v/v) ethanol as a co-solvent to obtain extracts rich in flavonoids and volatile organic compounds (VOCs) from Cordyceps sinensis. Almeida et al. [151] further reported that the volumetric proportion of ethanol used as a co-solvent was the most critical factor for enhancing ergosterol extraction yield from A. bisporus, albeit at the expense of reduced ergosterol purity in the resulting extract. As with other advanced extraction techniques, optimization of operational parameters, including pressure, temperature, extraction time, and CO2 flow rate, is essential to maximize SFE efficiency. In an investigation using different pressures and temperatures, for instance, Mazzutti et al. [159] identified optimal conditions for phenolic compounds extraction at 30.0 MPa and 323.15 K. Early studies, such as by Abdullah et al. [160], demonstrated the feasibility of using SC-CO2 alone to rapidly extract fatty and carboxylic acids from Agaricus spp. More recent investigations have focused on comparative performance and process efficiency relative to conventional methods.
Krivošija et al. [108] reported that a 4 h SC-CO2 extraction effectively recovered fatty acids and sterols from several mushroom species, including L. saccatum, P. ostreatus, and C. cibarius (Table 3). Although Soxhlet extraction (8 h) yielded slightly higher recoveries, the authors considered the difference negligible in view of the substantial advantages of SC-CO2, such as reduced solvent use and shorter processing time. Comparable findings were reported by Joradon et al. [161], who observed no significant differences in ergosterol and total polyphenol yields from H. erinaceus obtained via SC-CO2 (1 h, 46.38 °C, 100 bar) and conventional maceration (72 h). In contrast, Li et al. [162] demonstrated superior sterol recovery from G. lucidum spores using SC-CO2 at 35 MPa and 48 °C for 3 h with 20% ethanol as a co-solvent compared with Soxhlet extraction. Collectively, these findings highlight the versatility, efficiency, and sustainability of SFE for the recovery of pharmaceutical-grade bioactive compounds from edible mushrooms.
Pressurized Liquid Extraction (PLE)
Pressurized liquid extraction (PLE) is referred to in the literature by several interchangeable terms, including accelerated solvent extraction (ASE), enhanced solvent extraction, pressurized fluid extraction, accelerated fluid extraction, subcritical water extraction (SWE), and high-pressure solvent extraction (HPSE), all of which are based on the same operational principle. In PLE system, the extraction solvent is maintained at elevated temperatures and pressures, typically near its supercritical region. High temperatures enhance solute solubility and diffusion rates, while the applied pressure prevents solvent boiling, thereby preserving the liquid phase above its normal boiling point. This combination promotes disruption of the mushroom matrix and facilitates efficient solvent penetration and mass transfer [99,133].
Similar to other advanced extraction techniques, PLE achieves high extraction efficiencies within shorter processing times and with reduced solvent consumption compared with conventional methods (Table 3). The process is commonly automated (Table 1) and conducted in closed systems that limit exposure to oxygen and light, thereby reducing oxidative degradation of sensitive bioactive compounds [133]. Comparative studies highlight the superior performance of PLE for mushroom bioactives. For example, Hwang et al. [123] evaluated non-conventional (PLE, UAE, EAE) and conventional (hot-water) extraction methods for chaga mushroom (I. obliquus) and reported that PLE at 121 °C and 0.11–0.12 MPa produced the highest yields of β-glucans and total phenolics within 2 h. Similarly, Yang et al. [163] demonstrated that SWE (a specific form of PLE) doubled polysaccharide yields from G. frondosa in 43.65 min compared with hot-water extraction requiring 3 h.
Subcritical water extraction (SWE) employs water as the solvent and enables selective recovery of different classes of bioactive compounds by adjusting temperature. At lower temperatures, SWE preferentially extracts polar compounds, whereas higher temperatures (>100 °C) favor the extraction of less polar constituents due to reduced dielectric constant of water [101]. This means that elevating water above its boiling point under pressurized conditions enhances its ability to solubilize and extract less polar compounds that are otherwise poorly soluble under ambient aqueous conditions. Using this approach, Yang et al. [163] reported an optimal polysaccharide yield of 25.1% from G. frondosa at 210 °C. Extraction conditions strongly influence compound recovery, particularly for phenolic constituents, which generally require elevated temperatures. Krümmel et al. [103] observed a 27% increase in phenolic yield from P. sajor-caju using PLE at 80 °C compared with 40 °C at 10 MPa. Likewise, Sakdasri et al. [164] reported a 25.5% improvement in polyphenol recovery from the same edible mushroom at 140 °C relative to 100 °C using PLE. In addition to temperature, solvent pH can also affect extraction efficiency; Abu-Reidah et al. [165] found that the highest total phenolic content from I. obliquus was obtained at pH 11.5 and 100 °C. These studies collectively underscore the flexibility and effectiveness of PLE as a green and high-performance extraction strategy for pharmaceutical-relevant mushroom bioactives.
These advanced extraction technologies may also be applied in sequential or hybrid configurations to further enhance the recovery of bioactive compounds from edible mushrooms. For example, Zhao et al. [148] showed that EAE followed by UAE produced the highest protein yield (9.4%) from L. edodes, representing approximately a twofold increase compared with EAE alone (4.9%) and a substantial improvement over UAE alone (6.9%). Similarly, Zhang et al. [125] reported that polysaccharide yields from D. indusiata followed the order ultrasound–microwave-assisted extraction > UAE > MAE. The superior performance of the combined approach was attributed to the synergistic effects of acoustic cavitation and microwave irradiation, which collectively enhance cell wall disruption and mass transfer, thereby facilitating more efficient release of target compounds into the extraction solvent. As reflected in the representative studies summarized in Table 3, advanced extraction techniques applied to edible mushrooms demonstrate method- and condition-dependent variations in extraction efficiency, target specificity, and bioactive recovery, underscoring the importance of optimizing process parameters for maximal yield.

4.4. Isolation and Purification: Crude Extract to Defined Ingredient

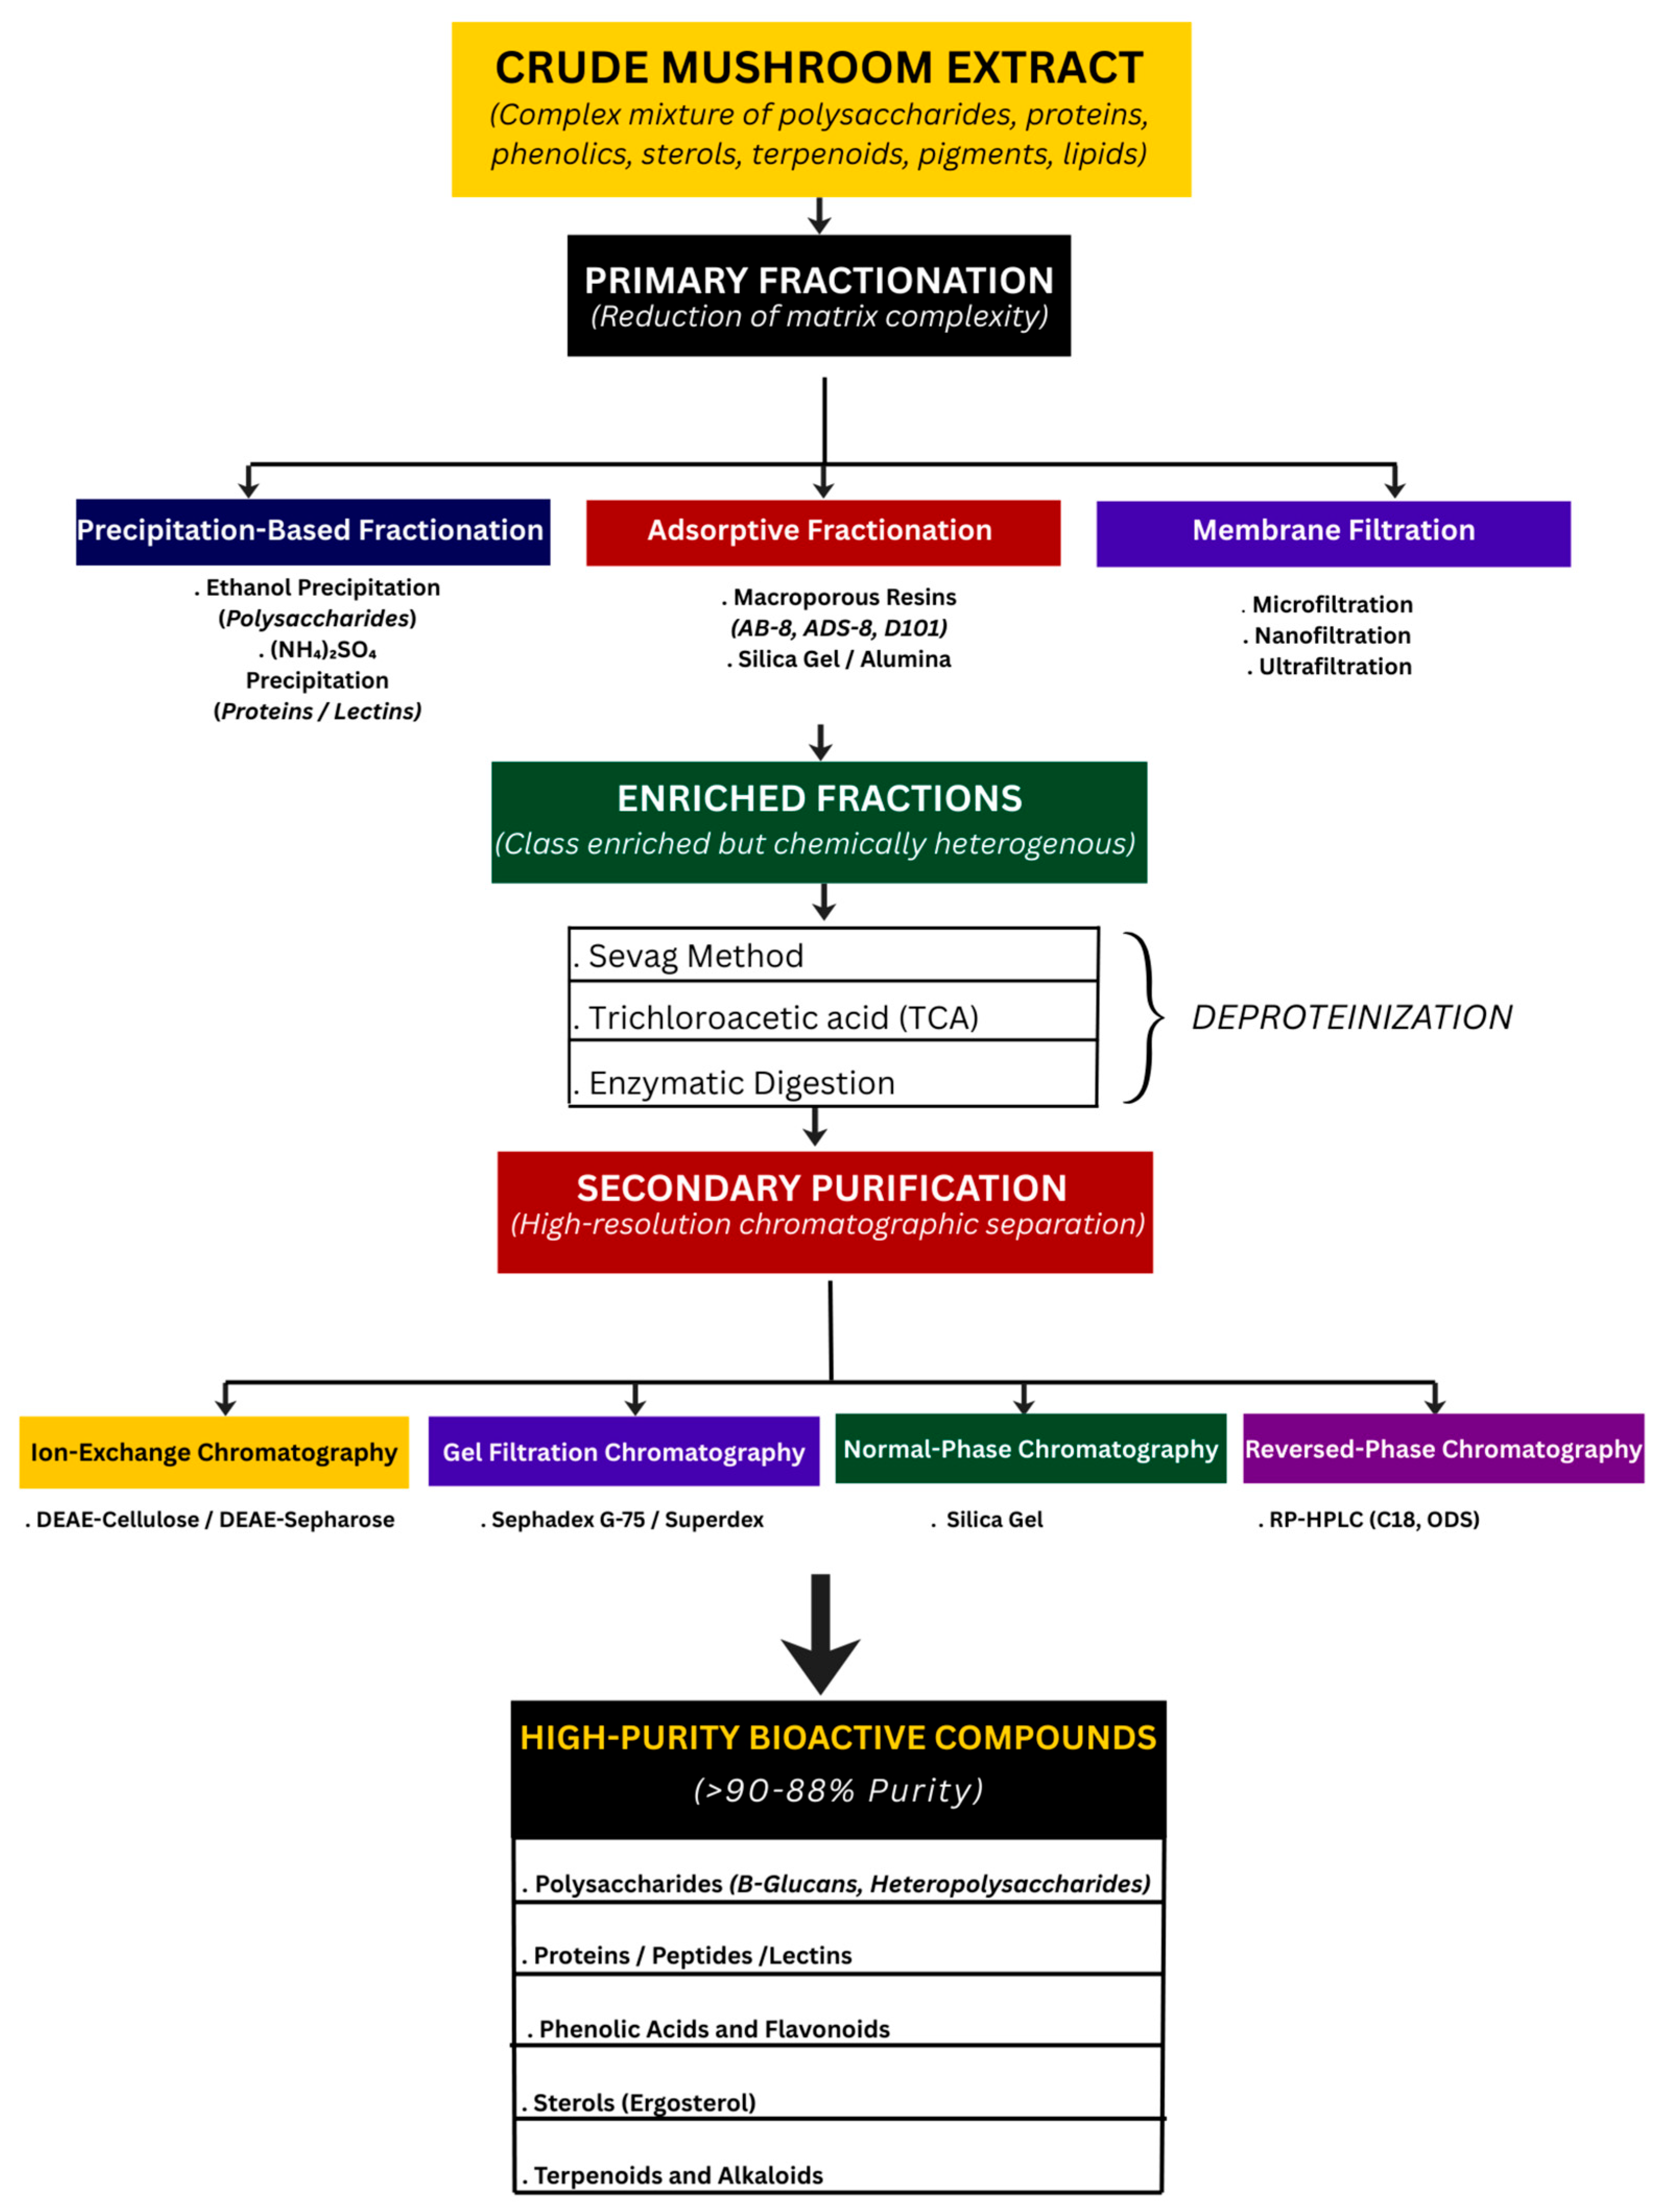
Crude extracts obtained from edible mushrooms using the extraction methods described above are complex matrices containing a wide range of co-extracted constituents. To obtain defined bioactive ingredients of pharmaceutical relevance, these extracts must undergo further isolation and purification (Figure 3). The presence of impurities can obstruct structural elucidation and compromise the biological activity of target compounds, emphasizing the need for this downstream processing to be effective [19].
High-resolution chromatographic techniques are commonly employed during the final stages of purification. However, because chromatographic media are costly and susceptible to fouling by residual protein and lipid impurities in the mushroom matrix, preliminary fractionation steps are typically applied to simplify the extract and reduce the contaminant load prior to chromatography. Widely used fractionation strategies include liquid–liquid partitioning, precipitation, adsorptive separation, and membrane filtration (Figure 3), owing to their operational simplicity, scalability, and cost-effectiveness [8,99].
Membrane filtration is a size-based separation technique classified into microfiltration, ultrafiltration, and nanofiltration according to membrane pore size [99]. It is extensively used in pharmaceutical processing to clarify extracts, concentrate target molecules, and remove low-molecular-weight impurities. Nevertheless, its selectivity is limited, as effective fractionation of proteins or polysaccharides requires substantial differences in molecular weight [8]. During membrane filtration, a semipermeable membrane selectively retains larger molecules while enabling the passage of smaller molecules. For example, Sari et al. [166] applied cross-flow ultrafiltration to crude L. edodes extracts, generating six fractions of distinct molecular sizes. Subsequent quantitative analysis of the fractions revealed trace levels of β-glucans and decreasing protein content with increasing fraction size. Similarly, Yang et al. [167] purified G. lucidum polysaccharides using a membrane with a 6 kDa molecular weight cut-off (MWCO), achieving a purity of 73.5% and a recovery rate of 69.4%. Using a high-performance ultrafiltration cell with 10, 3 and 1 kDa MWCO, Kaprasob et al. [168] also obtained four molecular size fractions (>10, 3–10, 1–3, and <1 kDa) of bioactive peptides from protein hydrolysate of B. edulis.
Adsorptive separation exploits differences in the affinity of extract components for solid adsorbents. The selection of an appropriate adsorbent as the stationary phase is critical to maximize recovery, ensure effective separation, and prevent irreversible adsorption of target compounds [99]. Common low-cost adsorbents include silica gel, macroporous resins, and alumina. Li et al. [169] demonstrated that ADS-8 resin exhibited superior adsorption and desorption capacities for the isolation of anticancer ganoderic acids GA-Mk and GA-T from G. lucidum mycelia. Concentrations of GA-Mk and GA-T increased from 45 and 22 mg/g in the crude extract to 352 and 141 mg/g, respectively, with recovery yields of 90.1% and 72.2%. In another study, Krüzselyi et al. [170] employed a two-step silica gel-based solid-phase extraction (SPE) approach to isolate minor bioactive constituents from P. citrinopileatus extracts rich in fatty acids. Thin-layer chromatography (TLC) confirmed a marked reduction in linoleic acid content in the eluate compared with the crude methanolic extract.
Graded ethanol precipitation is another widely applied fractionation method, particularly for polysaccharides, and is based on their differential solubility in aqueous ethanol solutions [19]. Increasing ethanol concentration reduces solvent polarity, promoting polysaccharide aggregation and precipitation, thereby yielding fractions enriched in the target compound. Additional deproteinization techniques, including the Sevag method, trichloroacetic acid treatment, and enzymatic digestion, are often employed to remove co-extracted proteins, with the Sevag method being the most commonly used (Figure 3) [18]. Barbosa et al. [105], for instance, precipitated polysaccharides from P. ostreatus crude extracts obtained by SFE–CO2 (with water as co-solvent) using three volumes of 95% ethanol at 4 °C for 24 h. The polysaccharide-rich fractions were subsequently deproteinized using the Sevag reagent (n-butanol/chloroform, 1:5 v/v) prior to structural analysis. Other edible mushrooms whose crude extracts have been fractionated for polysaccharides using ethanol precipitation and/or deproteinization include Phellinus linteus [171,172], C. versicolor, G. frondosa, G. lucidum and Antrodia cinnamomea [171], Morchella esculenta [173], D. indusiata [125], P. ostreatus and G. lucidum [155], Hypsizygus marmoreus [112], Armillaria mellea [141], P. eryngii [142], Pleurotus cystidiosus [174], L. velutinus [117] and C. sinensis mycelia [175]. Depigmentation of co-extracted colored impurities is another essential step in polysaccharide isolation and is commonly achieved using approaches such as polyamide resin adsorption, activated carbon treatment, or dialysis membrane separation [20]. Although such approaches yield relatively pure carbohydrate fractions, individual fractions may still comprise polysaccharides of varying molecular weights [133].
Salt-based precipitation techniques also play a role in fractionation. Ammonium sulfate [(NH4)2SO4] is frequently used for protein isolation. Mogahid et al. [176] reported the initial separation of a novel hemagglutination-inhibiting lectin from P. eryngii using 80% ammonium sulfate saturation. In addition, Liu et al. [177] combined quaternary ammonium salt precipitation (10% hexadecyltrimethylammonium bromide) with ultrafiltration of 10 kDa MWCO to purify crude polysaccharides (TLH-3) from Tricholoma lobayense. This integrated approach resulted in higher yields, larger processing volumes, and shorter purification times compared with conventional column chromatography.
Fractions obtained from preliminary fractionation often remain chemically complex, containing multiple constituents with closely related physicochemical properties. This complexity complicates the isolation of target bioactive compounds, particularly when structural analogs or isomers are present [8]. Consequently, column chromatography employing finely packed stationary phases (typically <5 μm) is widely adopted as the final step of isolating the target compound. High-performance liquid chromatography (HPLC), which operates under elevated pressure to drive the mobile phase through the column, is especially prevalent at the laboratory scale for the isolation of single, high-purity compounds on the basis of their polarity. For example, Naumoska et al. [178] developed a two-dimensional chromatographic strategy to isolate the neuroprotective compound erinacine A from crude H. erinaceus extract. This approach combined initial fractionation using normal-phase flash chromatography on silica with subsequent purification by semi-preparative reversed-phase HPLC (C18), yielding 19.4 mg of erinacine A with a chromatographic purity of 97.4%. In a similar study, Le et al. [179] repeatedly subjected the ethyl acetate fraction of Phellinus igniarius to silica gel column chromatography (600 g, 160 × 7 cm) to obtain an Inoscavin A-enriched fraction, which was subsequently purified by preparative HPLC using a Luna C18 column to yield Meshimakobnol A. These purified compounds were subsequently employed as reference standards for RP-HPLC–PDA-based quantitative analysis of the same constituents in other Phellinus species. Reversed-phase HPLC (HPLC-RP, C18) was also employed to separate the water-soluble, polar compound muscimol from the aqueous extract of Amanita muscaria [180].
Ion-exchange chromatography (IEC) and gel filtration chromatography, also referred to as size-exclusion chromatography (SEC), are among the most commonly applied chromatographic techniques, particularly for the purification of mushroom polysaccharides. IEC separates compounds based on differences in net surface charge, incorporating ion-exchange mechanisms with liquid chromatographic separation [181]. Bioactive components of edible mushrooms bearing ionizable functional groups can be selectively retained on charged resin beads and subsequently eluted by modifying the mobile-phase pH or ionic strength. Anion-exchange resins such as DEAE-agarose or DEAE-cellulose are typically used for neutral or acidic polysaccharides and phenolic compounds, whereas cation-exchange resins (e.g., sulfonate or carboxylate matrices) are suitable for alkaloids [99,181]. In contrast, gel filtration chromatography relies on the molecular-sieving properties of porous beads to separate constituents according to their hydrodynamic size or molecular weight [181]. Unlike membrane filtration, smaller molecules are retained longer within the pores of the stationary phase, while larger molecules elute earlier. Common stationary phases include Sephadex (cross-linked dextran), agarose gels, and polyacrylamide-based media (Bio-Gel P) [99].
These charge- and size-based chromatographic approaches have been effectively combined for polysaccharide purification across different species. Liu et al. [177] initially fractionated T. lobayense polysaccharides by DEAE ion-exchange chromatography to obtain TLH-1 and TLH-S fractions, followed by purification on a Superdex-75 gel filtration column (Cytiva, Wilmington, DE, UAS) (2.6 × 50 cm) to isolate the potent antioxidant polysaccharide TLH-3. However, when compared with a salt-precipitation–ultrafiltration strategy, the authors highlighted key limitations of column chromatography, including high separation-media (gel) costs, prolonged processing times (up to 8 days), and restricted sample loading capacity. These limitations emphasize the need to transition towards faster, more efficient and usually automated chromatographic processes, such as flash chromatography. Similarly, Luo et al. [182] purified a white mycelial polysaccharide (PBMP1) from P. baumii through sequential separation on a DEAE-cellulose-52 column (2.6 × 30 cm) followed by a Sephadex G-100 column (2.6 × 60 cm). Applying the same chromatographic sequence, Yang et al. [173] isolated a new polysaccharide (MEP-1) from hot-water extracts of M. esculenta using a DEAE-Cellulose A52 column (2.6 × 30 cm) and a Sephadex G-100 column (1.6 × 100 cm), achieving a yield of 1.58%. In a comparable study, Wang et al. [142] sequentially applied crude P. eryngii polysaccharides (PEP) to a DE-52 cellulose column (1.0 mL/min elution velocity) and a Sephadex G-100 column (0.25 mL/min), yielding a highly purified fraction (PEP-0.1-1) with a sugar content of 99.42%. Polysaccharides isolated from A. mellea and subsequently shown to exhibit significant antidiabetic activity in streptozotocin (STZ)-induced diabetic mice were purified using a DE-52 cellulose column (3.5 cm × 20 cm) [141]. Water-soluble polysaccharides from P. ostreatus were first separated from co-extracted proteins by exploiting electrostatic interactions on a DEAE-Sepharose Fast Flow column (43 × 1.5 cm), followed by further purification using Sephadex G-75 gel filtration chromatography (93 × 1.5 cm) [116].
Beyond polysaccharides, analogous multistep fractionation workflows have been employed for protein isolation from edible mushroom matrices. A bioactive protein (PEP) exhibiting anti-inflammatory activity was isolated from P. eryngii extracts through initial ammonium sulfate precipitation (60–80% saturation), succeeded by purification on a DEAE-Sepharose Fast Flow column, resulting in a product with >95% purity [183]. In another study, Lau et al. [184] employed graded ammonium sulfate precipitation (10–100% saturation) to concentrate proteins from a crude aqueous extract of A. bisporus. Protein precipitates that exhibited the highest ACE inhibitory activity were further fractionated by reversed-phase HPLC (HPLC-RP), and the active fractions were subsequently purified by gel filtration (Biosep SEC-S2000 column (Phenomenex, Torrance, CA, USA); 300 × 7.8 mm), yielding seven fractions with recovery rates ranging from 0.7% to 5.1%. Furthermore, Zhou et al. [185] fractionated Ramaria botrytis extracts by precipitation with 80% (NH4)2SO4, followed by sequential chromatographic purification of the crude protein on a DEAE–Sepharose Fast Flow column (2.0 × 40 cm) and a Superdex 75 10/300 size-exclusion column. This combined fractionation and chromatographic strategy led to the isolation of a ubiquitin-like antitumor protein (RBUP) with a yield of 9.43%.
In parallel with macromolecular purification, similar chromatographic principles have been extended to low-molecular-weight secondary metabolites. For instance, the ethyl acetate extract of Paxillus involutus was subjected to successive chromatographic separations, including silica gel column chromatography (200–300 mesh), octadecylsilane (ODS)-based semi-preparative reversed-phase HPLC (250 × 10 mm), and Sephadex LH-20 column chromatography. These techniques were applied iteratively to isolate rare 2,5-diarylcyclopentenone derivatives and to identify novel compounds designated as involutenones [121]. Similarly, Imam et al. [126] isolated anticancer metabolites, including indole-3-lactic acid, from aqueous L. edodes extracts through sequential purification involving silica gel column chromatography (230–400 mesh) followed by semi-preparative reversed-phase HPLC (C18). In a related study, Béni et al. [186] recovered four secondary metabolites, osmundalactone, 5-hydroxy-hex-2-en-4-olide (lactones), and the terphenyl quinones spiromentins C and B, from Tapinella atrotomentosa by subjecting its chloroform extract to flash silica gel column chromatography and subsequent normal-phase HPLC purification.
Collectively, these studies underscore that sequential fractionation and chromatographic purification are indispensable for obtaining mushroom-derived bioactives at high purity. Such purification workflows (Figure 3) constitute a controlled pipeline that inherently enables standardization, as each step is systematically monitored (e.g., by TLC) and analytically validated to ensure that the isolated compounds meet defined criteria for identity, purity, and bioactivity, thereby enabling the generation of reproducible, pharmaceutical-grade materials.

4.5. Structural Elucidation and Characterization

Following isolation and purification, rigorous structural elucidation and physicochemical characterization are essential for identification and purity validation of bioactive compounds derived from edible mushrooms. Structural characterization not only confirms molecular composition and architecture but also underpins structure–activity relationships (SAR), quality control, and regulatory acceptance in pharmaceutical development [17]. For example, Guo et al. [20] highlighted that the glycosidic linkages, branching degree, and molecular weight of Volvariella polysaccharides critically influence their physicochemical properties and biological activities. Similarly, the biological activities of proteins derived from edible mushrooms are strongly influenced by their molecular weight, amino acid composition, structural conformation, and peptide sequence [187].
Fully elucidated compounds further serve as molecular templates for the rational design or modification of related analogs aimed at optimizing biological performance [171]. Given the extensive chemical diversity of mushroom metabolites, including polysaccharides, proteins, terpenoids, phenolics, alkaloids, and sterols, no single analytical technique is sufficient for comprehensive structural resolution. Consequently, contemporary studies adopt integrated, multi-platform analytical strategies that combine chromatographic, spectroscopic, and spectrometric approaches to achieve unambiguous structural identification (Table 4). As summarized in Table 4, representative studies illustrate the structural features of bioactive compounds isolated from diverse edible mushroom species using these analytical tools.
Chromatographic techniques, particularly HPLC, are routinely employed to assess compound purity and homogeneity, especially for low-molecular-weight constituents such as triterpenoids. Mass spectrometry (MS), often coupled with liquid or gas chromatography (LC–MS, GC–MS), provides accurate molecular mass determination, elemental composition, fragmentation patterns, and insights into substitution and functional group arrangements. This technique operates by ionizing chemical species, followed by separating the resulting ions according to their mass-to-charge (m/z) ratios under vacuum conditions [113]. Coupling MS with chromatographic separation enhances its applicability to complex extracts and enables sensitive detection of bioactive compounds present at low concentrations [188]. Nuclear magnetic resonance (NMR) spectroscopy remains the cornerstone of definitive structural elucidation. By exploiting the magnetic properties of specific atomic nuclei, NMR provides detailed information on molecular connectivity, stereochemistry, and conformational features through one- and two-dimensional experiments. Its capacity to identify functional groups and distinguish between structural and stereochemical isomers makes NMR indispensable for natural product characterization. Nevertheless, its application is constrained by relatively low sensitivity and the requirement for highly purified, homogeneous samples [17,133]. In addition, NMR is resource-intensive, demanding both high investment and dedicated, specialized expertise.
For macromolecular bioactives such as polysaccharides and proteins, which exhibit hierarchical structural organization (primary, secondary, tertiary, and quaternary levels), additional analytical tools are required. These include size-exclusion chromatography (SEC), matrix-assisted laser desorption/ionization time-of-flight mass spectrometry (MALDI-TOF-MS), Fourier-transform infrared spectroscopy (FT-IR), circular dichroism (CD), X-ray diffraction (XRD), and amino acid sequencing (Table 4) [19]. For instance, Luo et al. [189] employed Size-Exclusion Chromatography with Multi-Angle Light Scattering and Refractive Index Detection (SEC–MALLS–RI) to identify a G. lucidum polysaccharide (GL-PWQ3) as highly branched with a compact, spherical conformation formed by stacked molecular chains. Similarly, Liu et al. [16], using scanning electron microscopy (SEM) and atomic force microscopy (AFM), demonstrated that branched polysaccharide chains from the same species (RGLP-1) intertwine to form circular aggregates. FT-IR spectroscopy is particularly valuable for rapid functional group identification and for probing molecular interactions and conformational changes relevant to biological activity [188]. Characteristic absorption bands at defined wavenumbers provide insights into structural motifs and bonding patterns [142].
Complementary techniques, including UV–visible (UV-Vis) spectroscopy, and optical rotation measurements, further support compound characterization, stability evaluation, and formulation development. These advanced analytical tools constitute a robust framework for the unambiguous identification and characterization of mushroom-derived bioactives, facilitating their translation from complex natural extracts into chemically defined, reproducible ingredients suitable for pharmaceutical innovation. A critical insight emerging from Table 4 is the recurrent lack of certain information across key characterization parameters, including molecular weight, precise monosaccharide or amino acid composition, definitive structural features, and, in some cases, bioactivity attribution. This pattern highlights substantial knowledge gaps in the comprehensive structural and functional elucidation of many mushroom-derived bioactives, despite their demonstrated biological potential. Notably, several studies report bioactivity without complete molecular definition, while others characterize chemical features without linking them to specific biological functions. These gaps present valuable research opportunities to apply these advanced analytical platforms in a more integrated manner to achieve full structure–activity relationships, standardize bioactive entities, and uncover novel mechanisms of action.

5. Critical Bottlenecks in Pharmaceutical Translation and Innovative Solutions

Despite substantial progress in the extraction, isolation, purification, and structural elucidation of mushroom-derived bioactives, significant hurdles remain before these compounds can achieve clinical and commercial success. Comprehensive molecular characterization in itself does not ensure biological reproducibility, scalable production, or clinical viability. Consequently, the translation of chemically well-defined mushroom bioactives into market-ready pharmaceutical ingredients is constrained by interconnected biological, technological, regulatory, and industrial challenges. This section therefore critically examines the principal bottlenecks limiting pharmaceutical translation and discusses emerging strategies aimed at bridging the gap between molecular characterization and real-world therapeutic application.
A major translational challenge is the poor oral bioavailability of many promising mushroom-derived compounds, particularly high-molecular-weight polysaccharides such as β-glucans. Comparative oral absorption studies indicate that β-glucans (>100 kDa) exhibit low systemic absorption, with reported bioavailability of only 2–5% [190], in contrast to triterpenoids from G. lucidum, which demonstrate moderate absorption levels of approximately 15–25% [191]. Nonetheless, triterpenoids, despite being lipophilic, face the complementary challenge of being rapidly metabolized via cytochrome P450 enzymes-mediated (CYP3A4) pathways and extensively bind to plasma proteins, leading to short effective half-lives of 2–4 h [192]. These pharmacokinetic limitations significantly restrict the efficacy of conventional oral formulations (e.g., tablets and capsules), which remain the preferred route of administration. From an industrial perspective, this necessitates either complex dosing strategies that may compromise patient compliance or substantial investment in advanced drug delivery systems, such as nano-encapsulation [192]. Nano-encapsulation has shown promise in enhancing compound stability and bioavailability; for instance, silver-based nanoparticles (AgNPs/He) synthesized using Hebeloma excedens extracts exhibited improved stability and bioaccessibility of phenolic compounds compared with crude mushroom extracts [193].
Another critical barrier to pharmaceutical translation is the lack of standardization and robust quality control frameworks, which are essential for the development of pharmaceutical-grade therapeutics. The absence of standardized practices severely limits reproducibility and impedes regulatory approval [192]. These challenges span the entire production pipeline, from variability in mushroom raw materials to inconsistencies in extraction and purification protocols. Biological heterogeneity in mushroom sourcing results in variable starting materials, while non-standardized extraction processes can lead to multi-fold differences in commercial products’ bioactive content. Furthermore, the high cost and limited availability of validated analytical methods constrain effective batch-to-batch consistency assessment for complex mushroom biomolecules [192,194]. Consequently, mushroom-based pharmaceutical products lacking rigorous quality control are prone to inconsistent therapeutic performance.
An additional complexity arises in defining the “active pharmaceutical ingredient” (API) for mushroom-derived preparations, particularly when bioactivity results from synergistic interactions among multiple constituents rather than a single compound [195]. Addressing this challenge requires the implementation of controlled cultivation systems compliant with Good Manufacturing Practice (GMP), coupled with genetic authentication strategies such as DNA barcoding to ensure species-level accuracy [196]. The implementation of GMP is complicated by biological variability arising from species differences, cultivation substrates, growth conditions, and post-harvest processing. These factors directly affect metabolite profiles and bioactivity, making batch-to-batch consistency particularly challenging for polysaccharides and crude extracts [194]. Given that toxicological evaluation in accordance with the guidelines of the International Council for Harmonisation of Technical Requirements for Pharmaceuticals for Human Use (ICH) is a critical step for pushing lead candidates toward pharmaceutical registration, impurity profiling constitutes a major regulatory hurdle [192]. Mushroom-derived products may contain residual proteins, endotoxins, heavy metals, pesticides, mycotoxins, or co-extracted secondary metabolites, all of which complicate toxicological characterization and safety assessment. Advanced analytical platforms, including LC–MS/MS fingerprinting combined with chemometric analyses, offer robust solutions for quality assurance and standardization; however, their widespread industrial adoption remains limited by high operational costs [192]. Another major challenge lies in the limited understanding of the mechanisms of action of many mushroom-derived compounds. Clear elucidation of the molecular pathways and signaling targets, through which these bioactive compounds interact with biological systems, is essential for rational drug design, dose optimization, and eventual regulatory approval [52].
More critically, the evidence base is limited by a scarcity of well-designed, randomized controlled human trials capable of defining safe and effective dosage ranges. Current knowledge therefore relies heavily on simplified in vitro systems and preclinical animal models, which often fail to adequately capture human pharmacokinetics, immune system complexity, and disease heterogeneity [5,192]. This translational gap arises from a convergence of aforementioned factors, including intrinsic pharmacokinetic constraints, poor bioavailability, model-dependent overestimation of efficacy, and the inherent difficulty of translating complex, multi-component mushroom extracts into standardized, regulatorily acceptable pharmaceutical entities. Collectively, these limitations help explain why robust preclinical findings have not consistently yielded clinical success. Nonetheless, the translational landscape is evolving, and mushroom-derived therapeutics are increasingly progressing toward clinical evaluation, with several edible mushroom-based formulations already assessed for bioactivity in phase I–III clinical trials (Table S1).
Finally, regulatory ambiguity remains a major barrier to the pharmaceutical development of mushroom-derived bioactives. Compounds intended for drug development must satisfy stringent and costly requirements, including extensive toxicological testing and human clinical evaluation, before qualification as Investigational New Drugs (INDs), in contrast to the less demanding regulatory pathways applied to dietary supplements. When marketed as dietary supplements, mushroom products are subject to relatively permissive regulatory frameworks that emphasize safety and labeling rather than demonstrated clinical efficacy. This burden, in combination with limited intellectual property protection for minimally modified natural compounds, frequently deters sustained industrial investment [196]. This challenge is further amplified by marked differences between European and American regulatory frameworks. In the European Union, the European Food Safety Authority (EFSA) applies a precautionary regulatory approach, particularly under the novel food and botanicals framework, which demands comprehensive compositional, toxicological, and human safety data, even for materials with a documented history of dietary use [197]. This process is often protracted and inflexible, especially for complex mushroom extracts whose bioactivity may arise from synergistic interactions rather than a single, well-defined API. By contrast, the United States Food and Drug Administration (FDA) provides a more clearly defined translational route through its Botanical Drug Development Guidance. This framework explicitly accommodates complex natural products, allowing progression as INDs provided batch consistency, chemical fingerprinting, and clinical safety are adequately demonstrated [197,198]. Although the FDA pathway still imposes rigorous quality and efficacy standards, its explicit recognition of “botanical drugs” category offers greater regulatory clarity and predictability [196].
Collectively, this regulatory asymmetry contributes to translational uncertainty and may help explain why mushroom-derived therapeutics more frequently advance through clinical development pipelines in the United States than in Europe. For instance, a comparative analysis by Calin et al. [199] showed that the US has conducted a markedly greater number of psilocybin (a tryptamine alkaloid derived from various mushroom genera) clinical trials, spanning both early- and late-stage development, than the EU. Addressing this imbalance will require greater harmonization and cross-recognition between regulatory frameworks, particularly through the development of clearer, internationally aligned pathways for complex natural products [197]. Establishing shared standards for quality control, safety evaluation, and characterization of multi-component extracts could reduce translational uncertainty, enhance global investment confidence, and facilitate more equitable advancement of mushroom-derived therapeutics across jurisdictions while maintaining rigorous safety and efficacy benchmarks.

6. Conclusions and Future Perspectives

Edible mushrooms represent a chemically rich and biologically versatile resource with considerable promise for pharmaceutical innovation. This review emphasizes that their therapeutic potential extends well beyond traditional nutraceutical applications, supported by a diverse repertoire of bioactive compounds with immunomodulatory, anticancer, antioxidant, anti-inflammatory, and cardioprotective properties. However, successful pharmaceutical translation requires a paradigm shift from bioactivity-driven discovery toward process-integrated development. A central conclusion of this review is that molecular characterization alone is insufficient to ensure clinical and industrial viability. Instead, reproducible biomass production, optimized extraction and purification workflows, rigorous structural elucidation, and robust quality control must be addressed as interconnected components of a unified development pipeline. The profound disconnect between strong preclinical evidence and limited clinical success does not reflect a lack of therapeutic promise, but rather unresolved challenges related to bioavailability, pharmacokinetics, model predictivity, standardization, and regulatory alignment. These constraints highlight the need for rational prioritization of mushroom-derived compounds based on criteria that extend beyond biological activity to include chemical definability, manufacturability, safety margins, and regulatory compatibility. Without such criteria, promising candidates remain difficult to advance as pharmaceutical-grade entities. The future of mushroom-based pharmaceuticals hinges on embracing interdisciplinary, innovative strategies. In addition to already outlined approaches, key research and development priorities include:
  • Integration of novel drug delivery strategies, including nano-formulations and encapsulation technologies, to protect compounds from degradation and enhance their targeted delivery.
  • Application of synthetic biology and metabolic engineering to sustainably produce high-value mushroom bioactives such as cordycepin, ergothioneine, and specific triterpenoids in yeasts or other microbial hosts using recombinant plasmids, thereby directly addressing sourcing and standardization challenges.
  • Deployment of omics technologies (genomics, transcriptomics, metabolomics) to identify novel compounds, refine structure–activity relationships and better unravel intricate molecular mechanisms associated with biosynthesis.
Overall, edible mushrooms occupy a strategic intersection between natural product chemistry and modern pharmaceutical science. With coordinated advances in biotechnology, analytical chemistry, and regulatory science, mushroom-derived bioactives are well positioned to contribute meaningfully to the next generation of natural-based pharmaceutical therapeutics.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/pr14050795/s1, Table S1. Representation of current landscape of clinical trials for edible mushrooms and their bioactive fractions.

Author Contributions

S.O.A., R.A.O. and C.G.A. conceived and designed the work; acquired, analyzed and interpreted the data, drafted the work or substantively revised it. S.O.A., R.A.O. and C.G.A. approved the submitted version. S.O.A., R.A.O. and C.G.A. agree to be personally accountable for the author’s own contributions and for ensuring that questions related to the accuracy or integrity of any part of the work, even ones in which the author was not personally involved, are appropriately investigated, resolved, and documented in the literature. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Data Availability Statement

No new data were created or analyzed in this study. Data sharing is not applicable to this article.

Acknowledgments

The authors acknowledge the technical support from Omolade Adesida on the manuscript figures.

Conflicts of Interest

The authors declare no conflicts of interest.

Abbreviations

ACEAngiotensin-Converting Enzyme
ASEAccelerated Solvent Extraction
APIActive Pharmaceutical Ingredient
CDCircular Dichroism
DEAEDiethylaminoethyl
EAEEnzyme-Assisted Extraction
EFSAEuropean Food Safety Authority
FIPFungal Immunomodulatory Protein
FT-IRFourier-Transform Infrared Spectroscopy
FDAUnited States Food and Drug Administration
GMPGood Manufacturing Practice
GC–MSGas Chromatography–Mass Spectrometry
HPLCHigh-Performance Liquid Chromatography
ICHInternational Council for Harmonisation of Technical Requirements for Pharmaceuticals for Human Use
IECIon-Exchange Chromatography
INDInvestigational New Drug
LC–MS/MSLiquid Chromatography–Tandem Mass Spectrometry
MALDI-TOF-MSMatrix-Assisted Laser Desorption/Ionization Time-of-Flight Mass Spectrometry
MAEMicrowave-Assisted Extraction
MWCOMolecular Weight Cut-Off
NMRNuclear Magnetic Resonance
PLEPressurized Liquid Extraction
PPCPolysaccharide-Protein Complex
SARStructure-Activity Relationship
SECSize-Exclusion Chromatography
SFESupercritical Fluid Extraction
SmFSubmerged Liquid Fermentation
SSFSolid-State Fermentation
SWESubcritical Water Extraction
TLCThin-Layer Chromatography
UAEUltrasound-Assisted Extraction
UV–VisUltraviolet-Visible Spectroscopy
XRDX-ray Diffraction

References

  1. Gupta, S.; Summuna, B.; Gupta, M.; Annepu, S.K. Edible Mushrooms: Cultivation, Bioactive Molecules, and Health Benefits. In Bioactive Molecules in Food; Mérillon, J.M., Ramawat, K., Eds.; Reference Series in Phytochemistry; Springer: Cham, Switzerland, 2018. [Google Scholar] [CrossRef] [Scilit]
  2. Adesida, S.O.; Alimba, C.G. Anticholesterol, Antihepatotoxic, and Immunomodulatory Activities of Bioactive Compounds of Edible Mushrooms. In Bioactive Compounds in Edible Mushrooms; Izah, S.C., Ogwu, M.C., Akram, M., Eds.; Reference Series in Phytochemistry; Springer: Cham, Switzerland, 2025; pp. 707–738. [Google Scholar] [CrossRef] [Scilit]
  3. Kumar, K.; Mehra, R.; Guiné, R.P.F.; Lima, M.J.; Kumar, N.; Kaushik, R.; Ahmed, N.; Yadav, A.N.; Kumar, H. Edible Mushrooms: A Comprehensive Review on Bioactive Compounds with Health Benefits and Processing Aspects. Foods 2021, 10, 2996. [Google Scholar] [CrossRef] [Scilit]
  4. Stabnikova, O.; Stabnikov, V.; Paredes-López, O. Wild and cultivated mushrooms as food, pharmaceutical and industrial products. Ukr. Food J. 2024, 13, 20–59. [Google Scholar] [CrossRef] [Scilit]
  5. Venturella, G.; Ferraro, V.; Cirlincione, F.; Gargano, M.L. Medicinal Mushrooms: Bioactive Compounds, Use, and Clinical Trials. Int. J. Mol. Sci. 2021, 22, 634. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Romero, J.C.F.; Oprea, O.B.; Gaceu, L.; Más Diego, S.M.; Morris Quevedo, H.J.; Galindo Alonso, L.; Rivero Ramírez, L.; Badea, M. Edible Mushroom Cultivation in Liquid Medium: Impact of Microparticles and Advances in Control Systems. Processes 2025, 13, 2452. [Google Scholar] [CrossRef] [Scilit]
  7. Arshadi, N.; Nouri, H.; Moghimi, H. Increasing the production of the bioactive compounds in medicinal mushrooms: An omics perspective. Microb. Cell Factories 2023, 22, 11. [Google Scholar] [CrossRef] [Scilit]
  8. Luo, H.; Li, Y. Downstream Processing of Medicinal Mushroom Products. In Biochemical Engineering and Biotechnology of Medicinal Mushrooms; Berovic, M., Zhong, J.J., Eds.; Springer: Cham, Switzerland, 2023; p. 184. [Google Scholar] [CrossRef] [Scilit]
  9. Yadav, D.; Negi, P.S. Bioactive components of mushrooms: Processing effects and health benefits. Food Res. Int. 2021, 148, 110599. [Google Scholar] [CrossRef] [Scilit]
  10. FAOSTAT. Food and Agriculture Organization of the United Nations Statistic. 2025. Available online: http://www.fao.org/faostat/en/#data (accessed on 9 December 2025).
  11. Sharma, E.; Bairwa, R.; Lal, P.; Pattanayak, S.; Chakrapani, K.; Poorvasandhya, R.; Kumar, A.; Altaf, M.A.; Tiwari, R.K.; Lal, M.K.; et al. Edible mushrooms trending in food: Nutrigenomics, bibliometric, from bench to valuable applications. Heliyon 2024, 10, e36963. [Google Scholar] [CrossRef] [Scilit]
  12. Rijia, A.; Krishnamoorthi, R.; Kaviyadharshini, M.; Mahalingam, P.U. Unlocking fungal fortunes: Cutting-edge extraction techniques and therapeutic possibilities of mushroom bioactive compounds. Food Chem. Adv. 2025, 6, 100895. [Google Scholar] [CrossRef] [Scilit]
  13. Parí, S.M.; Saldaña, E.; Rios-Mera, J.D.; Quispe Angulo, M.F.; Huaman-Castilla, N.L. Emerging Technologies for Extracting Antioxidant Compounds from Edible and Medicinal Mushrooms: An Efficient and Sustainable Approach. Compounds 2025, 5, 29. [Google Scholar] [CrossRef] [Scilit]
  14. Li, F.; Liu, T.; Liu, X.; Han, C.; Li, L.; Zhang, Q.; Sui, X. Ganoderma lucidum polysaccharide hydrogel accelerates diabetic wound healing by regulating macrophage polarization. Int. J. Biol. Macromol. 2024, 260, 129682. [Google Scholar] [CrossRef] [Scilit]
  15. Badalyan, S.M.; Barkhudaryan, A.; Rapior, S. Recent Progress in Research on the Pharmacological Potential of Mushrooms and Prospects for Their Clinical Application. In Medicinal Mushrooms; Agrawal, D., Dhanasekaran, M., Eds.; Springer: Singapore, 2019. [Google Scholar] [CrossRef] [Scilit]
  16. Liu, G.; Zhang, J.; Kan, Q.; Song, M.; Hou, T.; An, S.; Lin, H.; Chen, H.; Hu, L.; Xiao, J.; et al. Extraction, Structural Characterization, and Immunomodulatory Activity of a High Molecular Weight Polysaccharide From Ganoderma lucidum. Front. Nutr. 2022, 9, 846080. [Google Scholar] [CrossRef] [Scilit]
  17. Zhong, Y.; Tan, P.; Lin, H.; Zhang, D.; Chen, X.; Pang, J.; Mu, R. A Review of Ganoderma lucidum Polysaccharide: Preparations, Structures, Physicochemical Properties and Application. Foods 2024, 13, 2665. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Yin, Y.; Shi, X.; Cai, X.; Liu, F.; Ni, W.; Li, B.; Wan, X.; Ren, M. Isolation Techniques, Structural Characteristics, and Pharmacological Effects of Phellinus Polysaccharides: A Review. Molecules 2024, 29, 3047. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Wu, R.N.; Zhu, Y.Y.; Ma, R.H.; Ni, Z.J.; Deng, X.J.; Thakur, K.; Wei, Z.J. Purification, Structural Characteristics, Bioactive Properties, and Applications of Naematelia aurantialba Polysaccharides: A Comprehensive Review. Molecules 2025, 30, 4073. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Guo, L.; Wang, J.; Liu, H.; Zhang, H.; Mehaya, F.; Ma, C. Volvariella polysaccharides: Isolation, structural characterization and structure-activity relationship: A review. J. Future Foods 2026, 6, 161–172. [Google Scholar] [CrossRef] [Scilit]
  21. Zeb, M.; Lee, C.H. Medicinal Properties and Bioactive Compounds from Wild Mushrooms Native to North America. Molecules 2021, 26, 251. [Google Scholar] [CrossRef] [Scilit]
  22. Ferreira, I.C.; Vaz, J.A.; Vasconcelos, M.H.; Martins, A. Compounds from wild mushrooms with antitumor potential. Anti-Cancer Agents Med. Chem. 2010, 10, 424–436. [Google Scholar] [CrossRef] [Scilit]
  23. Barros, L.; Cruz, T.; Baptista, P.; Estevinho, L.M.; Ferreira, I.C. Wild and commercial mushrooms as source of nutrients and nutraceuticals. Food Chem. Toxicol. 2008, 46, 2742–2747. [Google Scholar] [CrossRef] [Scilit]
  24. Mattilda, P.; Könkö, K.; Eurola, M.; Pihlava, J.M.; Astola, J.; Vahteristo, L.; Hietaniemi, V.; Kumpulainen, J.; Valtonen, M.; Piironen, V. Contents of vitamins, mineral elements, and some phenolic compounds in cultivated mushrooms. J. Agric. Food Chem. 2001, 49, 2343–2348. [Google Scholar] [CrossRef] [Scilit]
  25. Zhang, Y.; Liu, W.; Xu, C.; Huang, W.; He, P. Characterization and Antiproliferative Effect of Novel Acid Polysaccharides from the Spent Substrate of Shiitake Culinary-Medicinal Mushroom Lentinus edodes (Agaricomycetes) Cultivation. Int. J. Med. Mushrooms 2017, 19, 395–403. [Google Scholar] [CrossRef] [Scilit]
  26. Wang, J.; Zhao, Y.; Li, W.; Wang, Z.; Shen, L. Optimization of polysaccharides extraction from Tricholoma mongolicum Imai and their antioxidant and antiproliferative activities. Carbohydr. Polym. 2015, 131, 322–330. [Google Scholar] [CrossRef] [Scilit]
  27. Fan, L.P.; Li, J.W.; Deng, K.Q.; Ai, L.Z. Effects of drying methods on the antioxidant activities of polysaccharides extracted from Ganoderma lucidum. Carbohydr. Polym. 2012, 87, 1849–1854. [Google Scholar] [CrossRef] [Scilit]
  28. Maity, P.; Sen, I.K.; Maji, P.K.; Paloi, S.; Devi, K.S.; Acharya, K.; Maiti, T.K.; Islam, S.S. Structural, immunological, and antioxidant studies of β-glucan from edible mushroom Entoloma lividoalbum. Carbohydr. Polym. 2015, 123, 350–358. [Google Scholar] [CrossRef] [Scilit]
  29. de Jesus, L.I.; Smiderle, F.R.; Cordeiro, L.M.C.; de Freitas, R.A.; Van Griensven, L.J.L.D.; Iacomini, M. Simple and effective purification approach to dissociate mixed water-insoluble α- and β-D-glucans and its application on the medicinal mushroom Fomitopsis betulina. Carbohydr. polym. 2018, 200, 353–360. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Valverde, M.E.; Hernández-Pérez, T.; Paredes-López, O. Edible mushrooms: Improving human health and promoting quality life. Int. J. Microbiol. 2015, 2015, 376387. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  31. Chan, G.C.F.; Chan, W.K.; Sze, D.M.Y. The effects of β-glucan on human immune and cancer cells. J. Hematol. Oncol. 2009, 2, 25–35. [Google Scholar] [CrossRef] [Scilit]
  32. De Sousa Cardozo, F.T.G.; Camelini, C.M.; Leal, P.C.; Kratz, J.M.; Nunes, R.J.; de Mendonça, M.M.; Simões, C.M.O. Antiherpetic mechanism of a sulfated derivative of Agaricus brasiliensis fruiting bodies polysaccharide. Intervirology 2014, 57, 375–383. [Google Scholar] [CrossRef] [Scilit]
  33. Su, C.H.; Lu, M.K.; Lu, T.J.; Lai, M.N.; Ng, L.T. A (1→6)-Branched (1→4)-β-d-Glucan from Grifola frondosa Inhibits Lipopolysaccharide-Induced Cytokine Production in RAW264.7 Macrophages by Binding to TLR2 Rather than Dectin-1 or CR3 Receptors. J. Nat. Prod. 2020, 83, 231–242. [Google Scholar] [CrossRef] [Scilit]
  34. He, X.; Lu, J.L.; Liao, W.F.; Long, Y.R.; Zhang, X.; Zhu, Q.; Lu, H.-L.; Hao, G.-Y.; Ding, K.; Sun, J.-H.; et al. GFPBW1, a β glucan from Grifola frondosa as vaccine adjuvant: APCs activation and maturation. Acta Pharmacol. Sin. 2024, 45, 2394–2404. [Google Scholar] [CrossRef] [Scilit]
  35. Jędrzejewski, T.; Pawlikowska, M.; Sobocińska, J.; Wrotek, S. Protein-Bound Polysaccharides from Coriolus versicolor Fungus Disrupt the Crosstalk Between Breast Cancer Cells and Macrophages through Inhibition of Angiogenic Cytokines Production and Shifting Tumour-Associated Macrophages from the M2 to M1 Subtype. Cell. Physiol. Biochem. 2020, 54, 615–628. [Google Scholar] [CrossRef] [Scilit]
  36. Phan, C.W.; David, P.; Tan, Y.; Naidu, M.; Wong, K.-H.; Kuppusamy, U.R.; Sabaratnam, V. Intrastrain comparison of the chemical composition and antioxidant activity of an edible mushroom, Pleurotus giganteus and its potent neuritogenic properties. Sci. World J. 2014, 378651, 1–10. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Phan, C.W.; Wang, J.K.; Cheah, S.C.; Naidu, M.; David, P.; Sabaratnam, V. A review on the nucleic acid constituents in mushrooms: Nucleobases, nucleosides and nucleotides. Crit. Rev. Biotech. 2018, 38, 762–777. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Ranogajec, A.; Beluhan, S.; Smit, Z. Analysis of nucleosides and monophosphate nucleotides from mushrooms with reversed-phase HPLC. J. Sep. Sci. 2010, 33, 1024–1033. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Yang, F.Q.; Lv, R.; Zhanga, Y.; Xia, Z. Comparison study on nucleosides and nucleotides in edible mushroom species by capillary zone electrophoresis. Anal. Methods 2012, 4, 546–549. [Google Scholar] [CrossRef] [Scilit]
  40. Chen, F.; Zhang, F.; Yang, N.; Liu, X. Simultaneous determination of 10 nucleosides and nucleobases in Antrodia camphorata using QTRAP LC-MS/MS. J. Chromatogr. Sci. 2014, 52, 852–861. [Google Scholar] [CrossRef] [Scilit]
  41. Ashraf, S.A.; Elkhalifa, A.E.O.; Siddiqui, A.J.; Patel, M.; Awadelkareem, A.M.; Snoussi, M.; Ashraf, M.S.; Adnan, M.; Hadi, S. Cordycepin for Health and Wellbeing: A Potent Bioactive Metabolite of an Entomopathogenic Medicinal Fungus Cordyceps with Its Nutraceutical and Therapeutic Potential. Molecules 2020, 25, 2735. [Google Scholar] [CrossRef] [Scilit]
  42. Zhou, C.; Yu, Z.; Chen, T.; Chen, Q.; Zhang, Y.; Cai, J.; Xu, C.; Yu, L. Tanshinone IIA attenuates cerebral-ischemia-reperfusion-induced neuroinflammation by inhibiting the TLR4/NF-κB signaling cascade: A study integrating network pharmacology, bioinformatics, and experimental validation. Phytomedicine 2025, 149, 157548. [Google Scholar] [CrossRef] [Scilit]
  43. Landi, N.; Clemente, A.; Pedone, P.V.; Ragucci, S.; Di Maro, A. An Updated Review of Bioactive Peptides from Mushrooms in a Well-Defined Molecular Weight Range. Toxins 2022, 14, 84. [Google Scholar] [CrossRef] [Scilit]
  44. Sousa, A.S.; Araújo-Rodrigues, H.; Pintado, M.E. The health-promoting potential of edible mushroom proteins. Curr. Pharm. Des. 2023, 29, 804–823. [Google Scholar] [CrossRef] [Scilit]
  45. El-Maradny, Y.A.; El-Fakharany, E.M.; Abu-Serie, M.M.; Hashish, M.H.; Selim, H.S. Lectins purified from medicinal and edible mushrooms: Insights into their antiviral activity against pathogenic viruses. Int. J. Biol. Macromol. 2021, 179, 239–258. [Google Scholar] [CrossRef] [Scilit]
  46. Singh, R.S.; Kaur, H.P.; Kanwar, J.R. Mushroom Lectins as Promising Anticancer Substances. Curr. Protein Pept. Sci. 2016, 17, 797–807. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Lin, C.H.; Sheu, G.T.; Lin, Y.W.; Yeh, C.-S.; Huang, Y.-H.; Lai, Y.-C.; Chang, J.-G.; Ko, J.-L. A new immunomodulatory protein from Ganoderma microsporum inhibits epidermal growth factor mediated migration and invasion in A549 lung cancer cells. Process Biochem. 2010, 45, 1537–1542. [Google Scholar] [CrossRef] [Scilit]
  48. Hsiao, Y.M.; Huang, Y.L.; Tang, S.C.; Shieh, G.J.; Lai, J.Y.; Wang, P.H.; Ying, T.H.; Ko, J.L. Effect of a Fungal immunomodulatory protein from Ganoderma tsugae on cell cycle and interferon gamma production through phosphatidylinositol 3-kinase signal pathway. Process Biochem. 2008, 43, 423–430. [Google Scholar] [CrossRef] [Scilit]
  49. Hsu, H.Y.; Hua, K.F.; Wu, W.C.; Hsu, J.; Weng, S.T.; Lin, T.L.; Liu, C.Y.; Hseu, R.S.; Huang, C.T. Reishi immuno-modulation protein induces interleukin-2 expression via protein kinase-dependent signaling pathways within human T cells. J. Cell Physiol. 2008, 215, 15–26. [Google Scholar] [CrossRef] [Scilit]
  50. Mariga, A.M.; Yang, W.J.; Mugambi, D.K.; Pei, F.; Zhao, L.Y.; Shao, Y.N.; Hu, Q. Antiproliferative and immunostimulatory activity of a protein from Pleurotus eryngii. J. Sci. Food Agric. 2014, 94, 3152–3162. [Google Scholar] [CrossRef] [Scilit]
  51. Qi, W.; Zhang, Y.; Yan, Y.B.; Lei, W.; Wu, Z.X.; Liu, N.; Liu, S.; Shi, L.; Fan, Y. The protective effect of cordymin, a peptide purified from the medicinal mushroom Cordyceps sinensis, on diabetic osteopenia in alloxan-induced diabetic rats. eCAM 2013, 2013, 985636. [Google Scholar] [CrossRef] [Scilit]
  52. Mayirnao, H.S.; Sharma, K.; Jangir, P.; Kaur, S.; Kapoor, R. Mushroom-derived nutraceuticals in the 21st century: An appraisal and future perspectives. J. Future Foods 2025, 5, 342–360. [Google Scholar] [CrossRef] [Scilit]
  53. Taofiq, O.; Calhelha, R.C.; Heleno, S.; Barros, L.; Martins, A.; Santos Buelga, C.; Queiroz, M.; Ferreira, I. Contribution of phenolic acids to the anti-inflammatory activity of mushrooms: Screening in phenolic extracts, individual parent molecules, and synthesized glucuronated and methylated derivatives. Food Res. Int. 2015, 76, 821–827. [Google Scholar] [CrossRef] [Scilit]
  54. Alkan, S.; Uysal, A.; Kaşık, G.; Vlaisavljevic, S.; Berezni, S.; Zengin, G. Chemical characterization, antioxidant, enzyme inhibition, and antimutagenic properties of eight mushroom species: A comparative study. J. Fungi 2020, 6, 166. [Google Scholar] [CrossRef] [Scilit]
  55. Krishnamoorthy, D.; Sankaran, M. Modulatory effect of Pleurotus ostreatus on oxidant/antioxidant status in 7, 12-dimethylbenz (a) anthracene induced mammary carcinoma in experimental rats--A dose-response study. J. Cancer Res. Ther. 2016, 12, 386–394. [Google Scholar] [CrossRef] [Scilit]
  56. Ebrahimzadeh, M.A.; Nabavi, S.M.; Nabavi, S.F.; Eslami, S. Antioxidant and Free Radical Scavenging Activities of Culinary-Medicinal Mushrooms, Golden Chanterelle Cantharellus cibarius and Angel’s Wings Pleurotus porrigens. Int. J. Med. Mushrooms 2010, 12, 265–272. [Google Scholar] [CrossRef] [Scilit]
  57. Bahadori, M.B.; Sarikurkcu, C.; Yalcin, O.U.; Cengiz, M.; Gungor, H. Metal concentration, phenolics profiling, and antioxidant activity of two wild edible Melanoleuca mushrooms (M. cognata and M. stridula). Microchem. J. 2019, 150, 104172. [Google Scholar] [CrossRef] [Scilit]
  58. Palacios, I.; Lozano, M.; Moro, C.; D’aRrigo, M.; Rostagno, M.; Martínez, J.; García-Lafuente, A.; Guillamón, E.; Villares, A. Antioxidant properties of phenolic compounds occurring in edible mushrooms. Food Chem. 2011, 128, 674–678. [Google Scholar] [CrossRef] [Scilit]
  59. Lang, S.; Liu, L.; Li, Z.; Liu, S.; Liang, J.; Lu, L.; Wang, L. Untargeted metabolomics reveals phenolic compound dynamics during mung bean fermentation. Food Chem. X 2025, 23, 103189. [Google Scholar] [CrossRef] [Scilit]
  60. Sánchez, C. Bioactives from mushroom and their application. In Food Bioactives; Puri, M., Ed.; Springer: Cham, Switzerland, 2017; pp. 23–57. [Google Scholar] [CrossRef] [Scilit]
  61. Van, Q.; Nayak, B.N.; Reimer, M.; Jones, P.J.H.; Fulcher, R.G.; Rempel, C.B. Anti-inflammatory effect of Inonotus obliquus, Polygala senega L. and Viburnum trilobum in a cell screening assay. J. Ethnopharmacol. 2009, 125, 487–493. [Google Scholar] [CrossRef] [Scilit]
  62. Bharadwaj, S.; Lee, K.E.; Dwivedi, V.D.; Yadava, U.; Panwar, A.; Lucas, S.J.; Pandey, A.; Kang, S.G. Discovery of Ganoderma lucidum triterpenoids as potential inhibitors against Dengue virus NS2B-NS3 protease. Sci. Rep. 2019, 9, 19059. [Google Scholar] [CrossRef] [Scilit]
  63. Zhang, B.B.; Guan, Y.Y.; Hu, P.F.; Chen, L.; Xu, J.W. Production of bioactive metabolites by submerged fermentation of the medicinal mushroom Antrodia cinnamomea: Recent advances and future development. Crit. Rev. Biotechnol. 2019, 39, 541–554. [Google Scholar] [CrossRef] [Scilit]
  64. Lodi, R.S.; Jia, X.; Yang, P.; Peng, C.; Dong, X.; Han, J.; Liu, X.; Wan, L.; Peng, L. Whole genome sequencing and annotations of Trametes sanguinea ZHSJ. Sci. Data 2025, 12, 1460. [Google Scholar] [CrossRef] [Scilit]
  65. Cateni, F.; Gargano, M.L.; Procida, G.; Venturella, G.; Cirlincione, F.; Ferraro, V. Mycochemicals in wild and cultivated mushrooms: Nutrition and health. Phytochem. Rev. 2022, 21, 339–383. [Google Scholar] [CrossRef] [Scilit]
  66. Sillapachaiyaporn, C.; Nilkhet, S.; Ung, A.T.; Chuchawankul, S. Anti-HIV-1 protease activity of the crude extracts and isolated compounds from Auricularia polytricha. BMC Complement. Altern. Med. 2019, 19, 351. [Google Scholar] [CrossRef] [Scilit]
  67. Sarma, D.; Saha, A.K.; Datta, B.K. Bioactive compounds with special reference to anticancer property of oyster mushroom Pleurotus ostreatus. J. Pharmacogn. Phytochem. 2018, 7, 2694–2698. [Google Scholar]
  68. Kikuchi, T.; Motoyashiki, N.; Yamada, T.; Tanaka, T. Ergostane-type sterols from king trumpet mushroom (Pleurotus eryngii) and their inhibitory effects on aromatase. Int. J. Mol. Sci. 2017, 18, 2479. [Google Scholar] [CrossRef] [Scilit]
  69. Kikuchi, T.; Kitaura, K.; Katsumoto, A.; Tanaka, T.; Saito, Y. Three bisabolane-type sesquiterpenes from the edible mushroom Pleurotus eryngii. Fitoterapia 2018, 129, 108–113. [Google Scholar] [CrossRef] [Scilit]
  70. Kikuchi, T.; Isobe, M.; Uno, S.; Tanaka, T.; Saito, Y. Strophasterols E and F: Rearranged ergostane-type sterols from Pleurotus eryngii. Bioorg. Chem. 2019, 89, 103011. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  71. Tejedor-Calvo, E.; Morales, D.; Marco, P.; Sánchez-Mata, M.C.; Tardío, J. Screening of bioactive compounds in truffles and evaluation of pressurized liquid extractions to obtain fractions with biological activities. Food Res. Int. 2020, 132, 109054. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  72. Onifade, R.S.; Alimba, C.G.; Adenipekun, C.O.; Bakare, A.A. White rot fungus (Pleurotus pulmonarius) cultivated on lead contaminated rice straw induced haematotoxicity and lead accumulation in liver and kidney of Wistar rats. J. Drug Metabol. Toxicol. 2016, 7, 210. [Google Scholar] [CrossRef]
  73. Olatunji-Ojo, A.M.; Alimba, C.G.; Adenipekun, C.O.; Bakare, A.A. Experimental simulation of somatic and germ cell genotoxicity in male Mus musculus fed extracts of lead contaminated Pleurotus ostreatus (white rot fungi). Environ. Sci. Pollut. Res. 2020, 27, 19754–19763. [Google Scholar] [CrossRef] [Scilit]
  74. Anusiya, G.; Gowthama, P.U.; Yamini, N.V.; Sivarajasekar, N.; Rambabu, K.; Bharath, G.; Banat, F. A review of the therapeutic and biological effects of edible and wild mushrooms. Bioengineered 2021, 12, 11239–11268. [Google Scholar] [CrossRef] [Scilit]
  75. Chukwuka, K.S.; Adesida, S.O.; Alimba, C.G. Carcinogenic and non-carcinogenic risk assessment of consuming metal-laden wild mushrooms in Nigeria: Analyses from field based and systematic review studies. Environ. Anal. Health Toxicol. 2023, 38, e2023013. [Google Scholar] [CrossRef] [Scilit]
  76. Antunes, F.; Marçal, S.; Taofiq, O.; Morais, A.; Freitas, A.C.; Ferreira, I.; Pintado, M. Valorization of Mushroom By-Products as a Source of Value-Added Compounds and Potential Applications. Molecules 2020, 25, 2672. [Google Scholar] [CrossRef] [Scilit]
  77. Melanouri, E.; Dedousi, M.; Diamantopoulou, P. Cultivating Pleurotus ostreatus and Pleurotus eryngii mushroom strains on agro-industrial residues in solid-state fermentation. Part I: Screening for growth, endoglucanase, laccase and biomass production in the colonization phase. Carbon. Resour. Convers. 2022, 5, 61–70. [Google Scholar] [CrossRef] [Scilit]
  78. Balenzano, G.; Spagnoletta, A.; Lentini, G.; Brunetti, G.; De Mastro, F.; Rullo, M.; Pisani, L.; Cirlincione, F.; Gargano, M.L.; Cavalluzzi, M.M. Microwave-Assisted Extraction of Pleurotus Mushrooms Cultivated on ‘Nero di Troia’ Grape Pomace and Evaluation of the Antioxidant and Antiacetylcholinesterase Activities. J. Fungi 2025, 11, 783. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  79. Zervakis, G.I.; Koutrotsios, G. Solid-State Fermentation of Plant Residues and Agro-industrial Wastes for the Production of Medicinal Mushrooms. In Medicinal Plants and Fungi: Recent Advances in Research and Development; Agrawal, D., Tsay, H.S., Shyur, L.F., Wu, Y.C., Wang, S.Y., Eds.; Medicinal and Aromatic Plants of the World; Springer: Singapore, 2017; Volume 4. [Google Scholar] [CrossRef] [Scilit]
  80. Saldanha, A.; Gomes, L.C.; Pinela, J.; Coimbra, M.A.; Barros, L.; Dias, M.I.; Pereira, C. Sustainable Cultivation of Edible Mushrooms: Preserving Biodiversity and Ensuring Product Quality. Biol. Life Sci. Forum 2023, 27, 6. [Google Scholar] [CrossRef] [Scilit]
  81. Wang, J.; Jiang, Q.; Huang, Z.; Wang, Y.; Roubik, H.; Yang, K.; Cai, M.; Sun, P. Solid-State Fermentation of Soybean Meal with Edible Mushroom Mycelium to Improve Its Nutritional, Antioxidant Capacities and Physicochemical Properties. Fermentation 2023, 9, 322. [Google Scholar] [CrossRef] [Scilit]
  82. Nacha, J.; Chen, H.; Owatworakit, A.; Saharat, K.; Makeudom, A.; Chamyuang, S. Solid-State Fermentation of Riceberry Rice with Mushroom Mycelium for Enhanced Beta-Glucan Production and Health Applications. Molecules 2025, 30, 3879. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  83. Akter, A.; Klausen, S.J.; Romero-Soto, L.A.; Díaz, F.; Domínguez, H.; Xiong, S.; Strætkvern, K.O.; Martín, C. Comparative extraction of bioactive compounds from spent mushroom substrates of Lentinula edodes and Pleurotus ostreatus using subcritical water and pressurized ethanol. Ind. Crop. Prod. 2025, 235, 121750. [Google Scholar] [CrossRef] [Scilit]
  84. Letti, L.; Vítola, F.; Pereira, G.; Karp, S.; Medeiros, A.; Scopel Ferreira da Costa, E.; Bissoqui, L.; Soccol, C. Solid-State Fermentation for the Production of Mushrooms. In Current Developments in Biotechnology and Bioengineering; Elsevier: Amsterdam, The Netherlands, 2018; pp. 285–318. [Google Scholar] [CrossRef] [Scilit]
  85. Elisashvili, V. Submerged Cultivation of Medicinal Mushrooms: Bioprocesses and Products (Review). Int. J. Med. Mushrooms 2012, 14, 211–239. [Google Scholar] [CrossRef] [Scilit]
  86. Fazenda, M.L.; Seviour, R.; McNeil, B.; Harvey, L.M. Submerged culture fermentation of “higher fungi”: The macrofungi. Adv. Appl. Microbiol. 2008, 63, 33–103. [Google Scholar] [CrossRef] [Scilit]
  87. Krasnopolskaya, L.; Shuktueva, M.; Golyshkin, A.; Almyasheva, N.; Yarina, M. Optimization of the Nutrient Medium for Flammulina velutipes Submerged Biomass Production and Micromorphology of Its Mycelium. Fermentation 2021, 7, 180. [Google Scholar] [CrossRef] [Scilit]
  88. Perveen, I.; Bukhari, B.; Sarwar, A.; Aziz, T.; Koser, N.; Younis, H.; Ahmad, Q.-U.; Sabahat, S.; Tzora, A.; Skoufos, I. Applications and efficacy of traditional to emerging trends in lacto-fermentation and submerged cultivation of edible mushrooms. Biomass Conv. Bioref. 2024, 14, 29283–29302. [Google Scholar] [CrossRef] [Scilit]
  89. Díaz-Godínez, G.; Téllez-Téllez, M.; Sánchez, C.; Díaz, R. Characterization of the Solid-State and Liquid Fermentation for the Production of Laccases of Pleurotus Ostreatus. In Fermentation Processes; InTech: Vienna, Austria, 2017. [Google Scholar] [CrossRef] [Scilit]
  90. Papaspyridi, L.M.; Aligiannis, N.; Topakas, E.; Christakopoulos, P.; Skaltsounis, A.L.; Fokialakis, N. Submerged Fermentation of the Edible Mushroom Pleurotus ostreatus in a Batch Stirred Tank Bioreactor as a Promising Alternative for the Effective Production of Bioactive Metabolites. Molecules 2012, 17, 2714–2724. [Google Scholar] [CrossRef] [Scilit]
  91. Jiamworanunkul, S. Effective antioxidant production through submerged fermentation of edible mushrooms. Thai J. Pharm. Sci. 2019, 43, 213–218. [Google Scholar] [CrossRef] [Scilit]
  92. Sun, M.; Zhuang, Y.; Gu, Y.; Zhang, G.; Fan, X.; Ding, Y. A comprehensive review of the application of ultrasonication in the production and processing of edible mushrooms: Drying, extraction of bioactive compounds, and post-harvest preservation. Ultrason. Sonochem. 2024, 102, 106763. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  93. Liufang, Y.; Wu, Y.; Zhou, H.; Qu, H.; Yang, H. Recent Advances in the Application of Natural Products for Postharvest Edible Mushroom Quality Preservation. Foods 2024, 13, 2378. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  94. Zhang, H.N.; Liu, Y.; Zhang, H.L.; Wan, Q.Z.; Wang, Y.Q. Effect of different drying and grinding techniques on the physicochemical properties and biological activities of fungal polysaccharides. Food Med. Homol. 2025, 2, 9420045. [Google Scholar] [CrossRef] [Scilit]
  95. Gąsecka, M.; Siwulski, M.; Magdziak, Z.; Budzynska, S.; Stuper-Szablewska, K.; Niedzielski, P.; Mleczek, M. The effect of drying temperature on bioactive compounds and antioxidant activity of Leccinum scabrum (Bull.) gray and Hericium erinaceus (Bull.) Pers. J. Food Sci. Technol. 2020, 57, 513–525. [Google Scholar] [CrossRef] [Scilit]
  96. Wei, Y.; Du, X.; Guo, Y.; Chang, M.; Deng, B.; Liu, J.; Cao, J. Elucidation of physicochemical properties of polysaccharides extracted from Cordyceps militaris fruiting bodies with different drying treatments and their effects on ulcerative colitis in zebrafish. Fron. Nutr. 2022, 9, 980357. [Google Scholar] [CrossRef] [Scilit]
  97. Saroj, P.; Xiong, S. Extraction and Measurement of Ergosterol in Mushroom and Mushroom Substrate. In Fungi; Navarro Simarro, P., Ed.; Methods and Protocols in Food Science; Humana: New York, NY, USA, 2026. [Google Scholar] [CrossRef] [Scilit]
  98. Xiaokang, W.; Lyng, J.G.; Brunton, N.P.; Cody, L.; Jacquier, J.C.; Harrison, S.M.; Papoutsis, K. Monitoring the effect of different microwave extraction parameters on the recovery of polyphenols from shiitake mushrooms: Comparison with hot-water and organic-solvent extractions. Biotechnol. Rep. 2020, 27, e00504. [Google Scholar] [CrossRef] [Scilit]
  99. Zhang, Q.W.; Lin, L.G.; Ye, W.C. Techniques for extraction and isolation of natural products: A comprehensive review. BMC Chin. Med. 2018, 13, 20. [Google Scholar] [CrossRef] [Scilit]
  100. Bhadange, Y.A.; Carpenter, J.; Saharan, V.K.A. Comprehensive Review on Advanced Extraction Techniques for Retrieving Bioactive Components from Natural Sources. ACS Omega 2024, 9, 31274–31297. [Google Scholar] [CrossRef] [Scilit]
  101. Roselló-Soto, E.; Parniakov, O.; Deng, Q.; Ankit, P.; Mohamed, K. Application of Non-conventional Extraction Methods: Toward a Sustainable and Green Production of Valuable Compounds from Mushrooms. Food Eng. Rev. 2016, 8, 214–234. [Google Scholar] [CrossRef] [Scilit]
  102. Naviglio, D.; Scarano, P.; Ciaravolo, M.; Gallo, M. Rapid Solid-Liquid Dynamic Extraction (RSLDE): A Powerful and Greener Alternative to the Latest Solid-Liquid Extraction Techniques. Foods 2019, 8, 245. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  103. Krümmel, A.; Gonçalves Rodrigues, L.G.; Vitali, L.; Salvador Ferreira, S.R. Bioactive compounds from Pleurotus sajor-caju mushroom recovered by sustainable high-pressure methods. LWT 2022, 160, 113316. [Google Scholar] [CrossRef] [Scilit]
  104. Alkin, M.; Söğüt, E.; Seydim, A.C. Determination of bioactive properties of different edible mushrooms from Turkey. Food Meas. 2021, 15, 3608–3617. [Google Scholar] [CrossRef] [Scilit]
  105. Barbosa, J.R.; Freitas, M.M.S.; Oliveira, L.C.; Martins, L.H.S.; Almada-Vilhena, A.O.; Oliveira, R.M.; Pieczarka, J.C.; Brasil, D.D.S.B.; Carvalho Junior, R.N. Obtaining extracts rich in antioxidant polysaccharides from the edible mushroom Pleurotus ostreatus using binary system with hot water and supercritical CO2. Food Chem. 2020, 330, 127173. [Google Scholar] [CrossRef] [Scilit]
  106. Zhu, M.; Han, Y.; Hu, X.; Gong, C.; Ren, L. Ergothioneine Production by Submerged Fermentation of a Medicinal Mushroom Panus conchatus. Fermentation 2022, 8, 431. [Google Scholar] [CrossRef] [Scilit]
  107. Bolesławska, I.; Górna, I.; Sobota, M.; Bolesławska-Król, N.; Przysławski, J.; Szymanski, M.W. Mushrooms as a Source of Bioactive Compounds and Their Antioxidant Properties—Preliminary Studies. Foods 2024, 13, 2612. [Google Scholar] [CrossRef] [Scilit]
  108. Krivošija, S.; Nastic, N.; Karadžic, B.M.; Kovacevic, S.; Podunavac-Kuzmanovic, S.; Vidovic, S. Supercritical Extraction and Compound Profiling of Diverse Edible Mushroom Species. Foods 2025, 14, 107. [Google Scholar] [CrossRef] [Scilit]
  109. Petrovic, J.; Papandreou, M.; Glamoclija, J.; Ciric, A.; Baskakis, C.; Proestos, C.; Lamari, F.; Zoumpoulakis, P.; Soković, M. Different extraction methodologies and their influence on the bioactivity of the wild edible mushroom Laetiporus sulphureus (Bull.) Murrill. Food Funct. 2014, 5, 2948–2960. [Google Scholar] [CrossRef] [Scilit]
  110. Maeng, J.; Shahbaz, H.; Ameer, K.; Jo, Y.; Kwon, J. Optimization of Microwave-Assisted Extraction of Bioactive Compounds from Coriolus versicolor Mushroom Using Response Surface Methodology: MAE of Bioactive Compounds from Mushroom. J. Food Process Eng. 2017, 40, e12421. [Google Scholar] [CrossRef] [Scilit]
  111. Sevindik, M.; Gürgen, A.; Khassanov, V.T.; Bal, C. Biological Activities of Ethanol Extracts of Hericium erinaceus Obtained as a Result of Optimization Analysis. Foods 2024, 13, 1560. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  112. Oliveira, R.S.; Biscaia, S.M.P.; Bellan, D.L.; Viana, S.R.F.; Di-Medeiros Leal, M.C.; Vasconcelos, A.F.D.; Lião, L.M.; Trindade, E.S.; Carbonero, E.R. Structure elucidation of a bioactive fucomannogalactan from the edible mushroom Hypsizygus marmoreus. Carbohydr. Polym. 2019, 225, 115203. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  113. Deveci, E.; Çayan, F.; Tel-Çayan, G.; Duru, M. Structural characterization and determination of biological activities for different polysaccharides extracted from tree mushroom species. J. Food Biochem. 2019, 43, e12965. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  114. Oni, J.; Ferdinand, A.; Markson, A.; Egwu, C.A. GC-MS Analysis of Bioactive Compounds in Some Wild-Edible Mushrooms from Calabar, Southern Nigeria. Eur. J. Biol. Biotechnol. 2020, 1, 1–9. [Google Scholar] [CrossRef] [Scilit]
  115. Buruleanu, L.C.; Radulescu, C.; Georgescu, A.A.; Danet, F.A.; Olteanu, R.L.; Nicolescu, C.M.; Dulama, I.D. Statistical Characterization of the Phytochemical Characteristics of Edible Mushroom Extracts. Anal. Lett. 2018, 51, 1039–1059. [Google Scholar] [CrossRef] [Scilit]
  116. Baeva, E.; Bleha, R.; Lavrova, E.; Sushytskyi, L.; Čopíková, J.; Jablonsky, I.; Klouček, P.; Synytsya, A. Polysaccharides from Basidiocarps of Cultivating Mushroom Pleurotus ostreatus: Isolation and Structural Characterization. Molecules 2019, 24, 2740. [Google Scholar] [CrossRef] [Scilit]
  117. Udchumpisai, W.; Bangyeekhun, E. Purification, Structural Characterization, and Biological Activity of Polysaccharides from Lentinus velutinus. Mycobiology 2020, 48, 51–57. [Google Scholar] [CrossRef] [Scilit]
  118. Fogarasi, M.; Socaciu, M.I.; Sălăgean, C.D.; Ranga, F.; Fărcaș, A.C.; Socaci, S.A.; Socaciu, C.; Țibulcă, D.; Fogarasi, S.; Semeniuc, C.A. Comparison of Different Extraction Solvents for Characterization of Antioxidant Potential and Polyphenolic Composition in Boletus edulis and Cantharellus cibarius Mushrooms from Romania. Molecules 2021, 26, 7508. [Google Scholar] [CrossRef] [Scilit]
  119. Ang, W.X.; Sarasvathy, S.; Kuppusamy, U.R.; Sabaratnam, V.; Tan, S.H.; Wong, K.T.; Perera, D.; Ong, K.C. In vitro antiviral activity of medicinal mushroom Ganoderma neo-japonicum Imazeki against enteroviruses that caused hand, foot and mouth disease. Tropic. Biomed. 2021, 38, 239–247. [Google Scholar] [CrossRef] [Scilit]
  120. Pandey, A.T.; Pandey, I.; Kerkar, P.; Singh, M.P. Antimicrobial activity and mycochemical profile of methanol extract from Pleurotus flabellatus. Vegetos 2021, 34, 619–629. [Google Scholar] [CrossRef] [Scilit]
  121. Lv, J.H.; Yao, L.; Zhang, J.X.; Wang, L.A.; Zhang, J.; Wang, Y.P.; Xiao, S.Y.; Li, C.T.; Li, Y. Novel 2,5-Diarylcyclopentenone Derivatives from the Wild Edible Mushroom Paxillus involutus and Their Antioxidant Activities. J. Agric. Food Chem. 2021, 69, 5040–5048. [Google Scholar] [CrossRef] [Scilit]
  122. Boonsong, S.; Klaypradit, W.; Wilaipun, P. Antioxidant activities of extracts from five edible mushrooms using different extractants. Agric. Nat. Resour. 2016, 50, 89–97. [Google Scholar] [CrossRef] [Scilit]
  123. Hwang, A.Y.; Yang, S.C.; Kim, J.; Lim, T.; Cho, H.; Hwang, K.T. Effects of Non-Traditional Extraction Methods on Extracting Bioactive Compounds from Chaga Mushroom (Inonotus obliquus) Compared with Hot Water Extraction. LWT 2019, 110, 80–84. [Google Scholar] [CrossRef] [Scilit]
  124. Gebreyohannes, G.; Sbhatu, D.B. Wild Mushrooms: A Hidden Treasure of Novel Bioactive Compounds. Int. J. Anal. Chem. 2023, 2023, 6694961. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  125. Zhang, Y.; Lei, Y.; Qi, S.; Fan, M.; Zheng, S.; Huang, Q.; Lu, X. Ultrasonic-microwave-assisted Extraction for Enhancing Antioxidant Activity of Dictyophora indusiata Polysaccharides: The Difference Mechanisms between Single and Combined Assisted Extraction. Ultrason. Sonochem. 2023, 95, 106356. [Google Scholar] [CrossRef] [Scilit]
  126. Imam, K.M.S.U.; Xie, Y.; Liu, Y.; Wang, F.; Xin, F. Extraction, Isolation, and Identification of Cytotoxic Secondary Metabolites from Shiitake Mushroom 808 Lentinula edodes (Berk.). ACS Food Sci. Technol. 2021, 1, 551–558. [Google Scholar] [CrossRef] [Scilit]
  127. Enman, J.; Rova, U.; Berglund, K.A. Quantification of the bioactive compound eritadenine in selected strains of shiitake mushroom (Lentinus edodes). J. Agric. Food Chem. 2007, 55, 1177–1180. [Google Scholar] [CrossRef] [Scilit]
  128. Nguyen, G.T.N.; Nguyen, T.M. Effect of extraction conditions (temperature, pH and time) by cellulase on chemical properties of dried oyster mushroom (Pleurotus sajor-caju) extract. Food Res. 2021, 5, 351–358. [Google Scholar] [CrossRef] [Scilit]
  129. Lucia, L.H.; Noelia, F.F.; María, D.T.; Herminia, D. Update on potential of edible mushrooms: High-value compounds, extraction strategies and bioactive properties. Int. J. Food Sci. Technol. 2022, 57, 1378–1385. [Google Scholar] [CrossRef] [Scilit]
  130. Zhu, Y.; Li, Q.; Mao, G.; Zou, Y.; Feng, W.; Zheng, D.; Wang, W.; Zhou, L.; Zhang, T.; Yang, J.; et al. Optimization of enzyme-assisted extraction and characterization of polysaccharides from Hericium erinaceus. Carbohydr. Polym. 2014, 101, 606–613. [Google Scholar] [CrossRef] [Scilit]
  131. Quintero-Cabello, K.P.; Palafox-Rivera, P.; Lugo-Flores, M.A.; Gaitan-Hernandez, R.; González-Aguilar, G.A.; Silva-Espinoza, B.A.; Tortoledo-Ortiz, O.; Ayala-Zavala, J.F.; Monribot-Villanueva, J.L.; Guerrero-Analco, J.A. Contribution of bioactive compounds to the antioxidant capacity of the edible mushroom Neolentinus lepideus. Chem. Biodivers. 2021, 18, e2100085. [Google Scholar] [CrossRef] [Scilit]
  132. Gogoi, P.; Chutia, P.; Singh, P.; Mahanta, C.L. Effect of Optimized Ultrasound-Assisted Aqueous and Ethanolic Extraction of Pleurotus citrinopileatus Mushroom on Total Phenol, Flavonoids and Antioxidant Properties. J. Food Process Eng. 2019, 42, e13172. [Google Scholar] [CrossRef] [Scilit]
  133. Villares, A.; Mateo-Vivaracho, L.; Guillamón, E. Structural Features and Healthy Properties of Polysaccharides Occurring in Mushrooms. Agriculture 2012, 2, 452–471. [Google Scholar] [CrossRef] [Scilit]
  134. Cheung, Y.; Siu, K.; Wu, J. Kinetic Models for Ultrasound-Assisted Extraction of Water-Soluble Components and Polysaccharides from Medicinal Fungi. Food Bioproc. Technol. 2013, 6, 2659–2665. [Google Scholar] [CrossRef] [Scilit]
  135. Aguiló-Aguayo, I.; Walton, J.; Viñas, I.; Tiwari, B.K. Ultrasound assisted extraction of polysaccharides from mushroom by-products. LWT 2017, 77, 92–99. [Google Scholar] [CrossRef] [Scilit]
  136. Ma, J.; Qiao, Z.; Xiang, X. Optimisation of extraction procedure for black fungus polysaccharides and effect of the polysaccharides on blood lipid and myocardium antioxidant enzymes activities. Carbohydr. Polym. 2011, 84, 1061–1068. [Google Scholar] [CrossRef] [Scilit]
  137. Özyürek, M.; Bener, M.; Güçlü, K.; Apak, R. Antioxidant/antiradical properties of microwave-assisted extracts of three wild edible mushrooms. Food Chem. 2014, 157, 323–331. [Google Scholar] [CrossRef] [Scilit]
  138. Zhang, Z.; Lv, G.; Pan, H.; Fan, L. Optimisation of the microwave-assisted extraction process for six phenolic compounds in Agaricus blazei murrill. Int. J. Food Sci. Technol. 2012, 47, 24–31. [Google Scholar] [CrossRef] [Scilit]
  139. Li, J.H.; Zhu, Y.Y.; Gu, F.T.; Wu, J.Y. Efficient isolation of immunostimulatory polysaccharides from Lentinula edodes by autoclaving-ultrasonication extraction and fractional precipitation. Int. J. Biol. Macromol. 2023, 237, 124216. [Google Scholar] [CrossRef] [Scilit]
  140. Chen, X.; Fang, D.; Zhao, R.; Gao, J.; Kimatu, B.M.; Hu, Q.; Chen, G.; Zhao, L. Effects of ultrasound-assisted extraction on antioxidant activity and bidirectional immunomodulatory activity of Flammulina velutipes polysaccharide. Int. J. Biol. Macromol. 2019, 140, 505–514. [Google Scholar] [CrossRef] [Scilit]
  141. Li, X.; Zhu, J.; Wang, T.; Sun, J.; Guo, T.; Zhang, L.; Yu, G.; Xia, X. Antidiabetic activity of Armillaria mellea polysaccharides: Joint ultrasonic and enzyme assisted extraction. Ultrason. Sonochem. 2023, 95, 106370. [Google Scholar] [CrossRef] [Scilit]
  142. Wang, H.; Ma, S.; Mariga, M.A.; Hu, Q.; Xu, Q.; Su, A.; Ma, N.; Ma, Q. Structural characterization and anti-inflammatory activities of novel polysaccharides obtained from Pleurotus eryngii. Food Sci. Hum. Wellness 2024, 13, 3031–3042. [Google Scholar] [CrossRef] [Scilit]
  143. Aliaño-González, M.J.; Barea-Sepúlveda, M.; Espada-Bellido, E.; Ferreiro-González, M.; López-Castillo, J.G.; Palma, M.; Barbero, G.F.; Carrera, C. Ultrasound-Assisted Extraction of Total Phenolic Compounds and Antioxidant Activity in Mushrooms. Agronomy 2022, 12, 1812. [Google Scholar] [CrossRef] [Scilit]
  144. Nugraha, A.; Briliantama, A.; Harun, M.U.; Sing-Chung, L.; Tan, C.X.; Vuanghao, L.; Amir, H.; Widiastuti, S. Ultrasound-assisted extraction of phenolic compounds from ear mushrooms (Auricularia auricula-judae): Assessing composition and antioxidant activity during fruiting body development. AIMS Agric. Food 2024, 9, 1134–1150. [Google Scholar] [CrossRef] [Scilit]
  145. Latif, A.; Khan, M.I.; Latif, A.; Khan, U.M.; Mousavi Khaneghah, A.; Aadil, R.M. Enhancing Polyphenol Extraction from White Button Mushrooms Using Microwave-Assisted Extraction: A Response Surface Methodology Optimization Approach. Microchem. J. 2024, 203, 110876. [Google Scholar] [CrossRef] [Scilit]
  146. Khotchai, W.; Therdthai, N.; Ritthiruangdej, P. Effect of microwave-assisted extraction on quality and taste profiles of crude extracts from split gill mushroom. J. Agric. Food Res. 2024, 19, 101588. [Google Scholar] [CrossRef] [Scilit]
  147. Harun, M.; Palma, M.; Setyaningsih, W. Development and Validation of Microwave-assisted Extraction for Phenolic Compound Profiling in Diverse Oyster Mushrooms (Pleurotus spp.) Sourced from Various Geographical Regions. J. Agric. Food Res. 2025, 20, 101754. [Google Scholar] [CrossRef] [Scilit]
  148. Zhao, Z.C.; Zhu, Y.Y.; Gu, F.T.; Huang, L.X.; Liu, X.; Wu, J.Y. Sequential Enzymatic and Ultrasonic Extraction of Lentinula edodes Mushroom Proteins Leading to Enhanced Yield and Significant Immunoactivity. Food Bioprocess Technol. 2025, 18, 10446–10462. [Google Scholar] [CrossRef] [Scilit]
  149. Prandi, B.; Cigognini, I.M.; Faccini, A.; Zurlini, C.; Rodríguez, Ó.; Tedeschi, T. Comparative Study of Different Protein Extraction Technologies Applied on Mushrooms By-products. Food Bioprocess Technol. 2023, 16, 1570–1581. [Google Scholar] [CrossRef] [Scilit]
  150. You, S.W.; Šimora, V.; Ivanišová, E.; Jančo, I.; Chlebová, Z.; Ďúranová, H.; Gabríny, L.; Kačániová, M.; de Medeiros, F.G.; Hoskin, R.T.; et al. Bioactive and Antioxidant Potential Agaricus bisporus Extracts Obtained by Different Extraction Methods and UV-B Irradiation. Food Bioeng. 2025, 4, 113–124. [Google Scholar] [CrossRef] [Scilit]
  151. Almeida, C.; Manrique, Y.; Lopes, J.C.; Martins, F.; Dias, M. Recovery of ergosterol from Agaricus bisporus mushrooms via supercritical fluid extraction: A response surface methodology optimisation. Heliyon 2024, 10, e21943. [Google Scholar] [CrossRef] [Scilit]
  152. Mishra, J.; Khan, W.; Ahmad, S.; Misra, K. Supercritical carbon dioxide extracts of Cordyceps sinensis: Chromatographybased metabolite profiling and protective efficacy against hypobaric hypoxia. Fron. Pharm. 2021, 12, 628924. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  153. Milovanovic, I.; Zengin, G.; Maksimovic, S.; Tadic, V. Supercritical and ultrasound-assisted extracts from Pleurotus pulmonarius mushroom: Chemical profiles, antioxidative, and enzyme-inhibitory properties. J. Sci. Food Agric. 2021, 101, 2284–2293. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  154. Tejedor-Calvo, E.; García-Barreda, S.; Sánchez, S.; Morte, A.; Siles-Sánchez, M.D.L.N.; Soler-Rivas, C.; Santoyo, S.; Marco, P. Application of Pressurized Liquid Extractions to Obtain Bioactive Compounds from Tuber aestivum and Terfezia claveryi. Foods 2022, 11, 298. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  155. Smiderle, F.R.; Morales, D.; Gil-Ramírez, A.; de Jesus, L.I.; Gilbert-López, B.; Iacomini, M.; Soler-Rivas, C. Evaluation of microwave-assisted and pressurized liquid extractions to obtain β-d-glucans from mushrooms. Carbohydr. Polym. 2017, 156, 165–174. [Google Scholar] [CrossRef] [Scilit]
  156. Kaya, M.; Çam, M. Eritadenine: Pressurized liquid extraction from Lentinula edodes and thermal degradation kinetics. Sustain. Chem. Pharm. 2022, 29, 100809. [Google Scholar] [CrossRef] [Scilit]
  157. Rodríguez-Seoane, P.; Perez, M.; Ana, C.; Sinde, E.; Domínguez, H. Antiradical and functional properties of subcritical water extracts from edible mushrooms and from commercial counterparts. Int. J. Food Sci. Technol. 2022, 57, 1420–1428. [Google Scholar] [CrossRef] [Scilit]
  158. Yasuma, T.; Toda, M.; Kobori, H.; Tada, N.; D’Alessandro-Gabazza, C.N.; Gabazza, E.C. Subcritical Water Extracts from Agaricus blazei Murrill’s Mycelium Inhibit the Expression of Immune Checkpoint Molecules and Axl Receptor. J. Fungi 2021, 7, 590. [Google Scholar] [CrossRef] [Scilit]
  159. Mazzutti, S.; Ferreira, S.; Riehl, C.; Smania Junior, A.; Smania, F.; Martínez, J. Supercritical fluid extraction of Agaricus brasiliensis: Antioxidant and antimicrobial activities. J. Supercrit. Fluids. 2012, 70, 48–56. [Google Scholar] [CrossRef] [Scilit]
  160. Abdullah, M.I.; Young, J.C.; Games, D.E. Supercritical fluid extraction of carboxylic and fatty acids from Agaricus spp. mushrooms. J. Agric. Food Chem. 1994, 42, 718–722. [Google Scholar] [CrossRef] [Scilit]
  161. Joradon, P.; Rungsardthong, V.; Ruktanonchai, U.; Suttisintong, K.; Thumthanaruk, B.; Vatanyoopaisarn, S.; Uttapap, D.; Mendes, A.C. Extraction of Bioactive Compounds from Lion’s Mane Mushroom by-Product Using Supercritical CO2 Extraction. J. Supercrit. Fluids. 2024, 206, 106162. [Google Scholar] [CrossRef] [Scilit]
  162. Li, J.W.; Zhang, X.X.; Liu, Y.F. Supercritical carbon dioxide extraction of Ganoderma lucidum spore lipids. LWT-Food Sci. Technol. 2016, 70, 16–23. [Google Scholar] [CrossRef] [Scilit]
  163. Yang, L.; Qu, H.; Mao, G.; Zhao, T.; Li, F.; Zhu, B.; Zhang, B.; Wu, X. Optimization of subcritical water extraction of polysaccharides from Grifola frondosa using response surface methodology. Pharmacogn. Mag. 2013, 9, 120–129. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  164. Sakdasri, W.; Arnutpongchai, P.; Phonsavat, S.; Bumrungthaichaichan, E.; Sawangkeaw, R. Pressurized Hot Water Extraction of Crude Polysaccharides, β-Glucan, and Phenolic Compounds from Dried Gray Oyster Mushroom. LWT 2022, 168, 113895. [Google Scholar] [CrossRef] [Scilit]
  165. Abu-Reidah, I.M.; Critch, A.L.; Manful, C.F.; Rajakaruna, A.; Vidal, N.P.; Pham, T.H.; Cheema, M.; Thomas, R. Effects of pH and Temperature on Water under Pressurized Conditions in the Extraction of Nutraceuticals from Chaga (Inonotus obliquus) Mushroom. Antioxidants 2021, 10, 1322. [Google Scholar] [CrossRef] [Scilit]
  166. Sari, M.; Toepler, K.; Nickisch-Hartfiel, A.; Teusch, N.; Hambitzer, R. Cross-Flow Ultrafiltration Fractions of a Cold Aqueous Extract of the Shiitake Culinary-Medicinal Mushroom, Lentinus edodes (Agaricomycetes), Exhibit Apoptosis in Tumor Cells. Int. J. Med. Mushrooms. 2018, 20, 1107–11119. [Google Scholar] [CrossRef] [Scilit]
  167. Yang, Z.J.; Jiang, Y.B.; Ge, F.H.; Zhou, J.K.; Yu, S.C.; Yuan, Y.J. Purification of Ganoderma lucidum polysaccharide by ultrafitration technology. J. Chin. Med. Matr. 2009, 32, 126–129. [Google Scholar]
  168. Kaprasob, R.; Khongdetch, J.; Laohakunjit, N.; Selamassakul, O.; Kaisangsri, N. Isolation and characterization, antioxidant, and antihypertensive activity of novel bioactive peptides derived from hydrolysis of King Boletus mushroom. LWT 2022, 160, 113287. [Google Scholar] [CrossRef] [Scilit]
  169. Li, Y.B.; Wang, J.L.; Zhong, J.J. Recovery of ganoderic acids from Ganoderma lucidum mycelia by macroporous adsorption resins. Biotechnol. Bioproc E 2012, 17, 326–336. [Google Scholar] [CrossRef] [Scilit]
  170. Krüzselyi, D.; Ott, P.G.; Móricz, A.M. Two-step dual-layer SPE method to separate antibacterial and antioxidant mushroom compounds. Talanta Open. 2024, 9, 100304. [Google Scholar] [CrossRef] [Scilit]
  171. Su, C.H.; Lai, M.N.; Lin, C.C.; Ng, L.-T. Comparative characterization of physicochemical properties and bioactivities of polysaccharides from selected medicinal mushrooms. Appl. Microbiol. Biotechnol. 2016, 100, 4385–4393. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  172. Gao, N.; Zhang, W.; Hu, D.; Lin, G.; Wang, J.; Xue, F.; Wang, Q.; Zhao, H.; Dou, X.; Zhang, L. Study on Extraction, Physicochemical Properties, and Bacterio-Static Activity of Polysaccharides from Phellinus linteus. Molecules 2023, 28, 5102. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  173. Yang, H.; Yin, T.; Zhang, S. Isolation, Purification, and Characterization of Polysaccharides from Wide Morchella esculenta (L.) Pers. Int. J. Food Prop. 2015, 18, 1385–1390. [Google Scholar] [CrossRef] [Scilit]
  174. Bibhash, C.P.; Prasenjit, M.; Ashis, K.N.; Manabendra, P.; Dilip, M.; Soumitra, M.; Satyajit, T.; Somenath, R.; Krishnendu, A.; Syed, S.I. Heteroglycan of an edible Mushroom Pleurotus cystidiosus: Structural characterization and study of biological activities. Inter. J. Biol. Macromol. 2017, 95, 833–842. [Google Scholar] [CrossRef] [Scilit]
  175. Li, Z.; Chen, A.; Li, Z.; Qu, M.; Chen, H.; Yang, B.; Wang, Y. A novel and environmentally friendly bioprocess for separation and partial purification of polysaccharides from Cordyceps sinensis mycelia by an aqueous two-phase system. RSC Adv. 2017, 7, 37659–37665. [Google Scholar] [CrossRef] [Scilit]
  176. Mogahid, H.S.T.; Altıparmak, Ü.G.; Özsoy, N.; Kavlo, H.; Sağırlı, P.A. Anti-inflammatory activity of a novel lectin isolated from Pleurotus eryngii var. ferulae mushroom. İstanbul J. Pharm. 2024, 54, 195–204. [Google Scholar] [CrossRef] [Scilit]
  177. Liu, L.; Lu, Y.; Li, X.; Zhou, L.; Yang, D.; Wang, L.; Chen, Y. A novel process for isolation and purification of the bioactive polysaccharide TLH-3′ from Tricholoma lobayense. Process Biochem. 2015, 50, 1146–1151. [Google Scholar] [CrossRef] [Scilit]
  178. Naumoska, K.; Gregori, A.; Albreht, A. Two-Dimensional Chromatographic Isolation of High Purity Erinacine A from Hericium erinaceus. J. Fungi 2025, 11, 150. [Google Scholar] [CrossRef] [Scilit]
  179. Le, A.N.; Nguyen, T.N.; Dong, D.T.A. Development of RP HPLC-PDA method for simultaneous quantitative analysis of Inoscavin A and Meshimakobnol A and application on some Phellinus mushroom species. Food Sci. Nutr. 2024, 12, 3602–3611. [Google Scholar] [CrossRef] [Scilit]
  180. Avila, E.; Guevara, P.J. Development of a RP-HPLC Method for Separating and Quantifying Muscimol in Different Developmental Stages of the Fungus Amanita muscaria. J. Chem. 2020, 2020, 8859998. [Google Scholar] [CrossRef] [Scilit]
  181. Ge, F.; Chen, Y.; Wang, B.; Zhou, W.; Du, B.; Hou, L. Bioactive Polysaccharides from Hericium erinaceus: Extraction, Structure, Bioactivities, and Applications. Molecules 2025, 30, 1850. [Google Scholar] [CrossRef] [Scilit]
  182. Luo, J.; Wu, J.; Xu, Y.; Shao, H.; Huang, P. Isolation, purification, and structural elucidation of a water-soluble polysaccharide derived from Phellinus baumii Pilát mycelia. Heliyon 2024, 10, e38239. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  183. Yuan, B.; Zhao, L.; Rakariyatham, K.; Han, Y.; Gao, Z.; Muinde, K.B.; Hu, Q.; Xiao, H. Isolation of a novel bioactive protein from an edible mushroom Pleurotus eryngii and its anti-inflammatory potential. Food Func. 2017, 8, 2175–2183. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  184. Lau, C.C.; Abdullah, N.; Shuib, A.S.; Aminudin, N. Novel angiotensin I-converting enzyme inhibitory peptides derived from edible mushroom Agaricus bisporus (J.E. Lange) Imbach identified by LC–MS/MS. Food Chem. 2014, 148, 396–401. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  185. Zhou, R.; Han, Y.J.; Zhang, M.H.; Zhang, K.R.; Ng, T.B.; Liu, F. Purification and characterization of a novel ubiquitin-like antitumour protein with hemagglutinating and deoxyribonuclease activities from the edible mushroom Ramaria botrytis. AMB Expr. 2017, 7, 47. [Google Scholar] [CrossRef] [Scilit]
  186. Béni, Z.; Dékány, M.; Kovács, B.; Csupor-Löffler, B.; Zomborszki, Z.P.; Kerekes, E.; Szekeres, A.; Urbán, E.; Hohmann, J.; Ványolós, A. Bioactivity-Guided Isolation of Antimicrobial and Antioxidant Metabolites from the Mushroom Tapinella atrotomentosa. Molecules 2018, 23, 1082. [Google Scholar] [CrossRef] [Scilit]
  187. Li, H.; Gao, J.; Zhao, F.; Liu, X.; Ma, B. Bioactive Peptides from Edible Mushrooms—The Preparation, Mechanisms, Structure—Activity Relationships and Prospects. Foods 2023, 12, 2935. [Google Scholar] [CrossRef] [Scilit]
  188. Soleiman-Beigi, M.; Ghiasbeigi, E. A study to identify S-S and S-S-S bonds in organic compounds by mass spectrometry and ultraviolet and raman spectroscopy techniques. J. Sulfur. Chem. 2019, 40, 1–8. [Google Scholar] [CrossRef] [Scilit]
  189. Luo, H.J.; Zhang, Y.K.; Wang, S.Z.; Lin, S.Q.; Wang, L.F.; Lin, Z.X.; Lu, G.D.; Lin, D.M. Structural characterization and antioxidative activity for a glycopeptide from Ganoderma lucidum fruiting body. Int. J. Biol. Macromol. 2024, 261, 129793. [Google Scholar] [CrossRef] [Scilit]
  190. Dong, Q.Q.; Wu, Q.; Lu, Y.; Shi, Y.; Yang, K.D.; Xu, X.L.; Chen, W. Exploring β-glucan as a micro-nano system for oral delivery targeted the colon. Int. J. Biol. Macromol. 2023, 253, 127360. [Google Scholar] [CrossRef] [Scilit]
  191. Li, D.; Lin, Y.; Lv, X.; Wu, Y.; Han, C.; Cao, P.; Zhang, G.; Leng, A.; Zhou, J.; Wang, C. Triterpenoids from Ganoderma lucidum inhibit cytochrome P450 enzymes interfering with the metabolic process of specific clinical drugs. Front. Pharmacol. 2024, 15, 1485209. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  192. Xiaoying, M.; Peng, Z.; Hong, W.; Na, G.; Jun, X.; Ying, Z.; Xun, C.; Guoli, L. From functional foods to immunotherapeutic agents: Mechanistic insights into medicinal mushroom bioactives in chronic inflammation management. Front. Nutr. 2025, 12, 1725297. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  193. Okumus, E. Green synthesis of silver nanoparticles using Hebeloma excedens mushroom extract as a new source: Anti-lipid peroxidation, bioaccessibility and antidiabetic properties. J. Food Meas. 2024, 18, 5157–5169. [Google Scholar] [CrossRef] [Scilit]
  194. Kour, H.; Kour, D.; Kour, S.; Singh, S.; Hashmi, S.A.J.; Yadav, A.N.; Kumar, K.; Sharma, Y.P.; Ahluwalia, A.S. Bioactive compounds from mushrooms: Emerging bioresources of food and nutraceuticals. Food Biosci. 2022, 50, 102124. [Google Scholar] [CrossRef] [Scilit]
  195. Wasser, S.P. Medicinal mushroom science: Current perspectives, advances, evidences, and challenges. Biomed. J. 2014, 37, 345–356. [Google Scholar] [CrossRef] [Scilit]
  196. Tokul-Ölmez, Ö.; Kaplaner, E.; Öztürk, M. Impact of Collection Locations and Host Trees on the Bioactive Triterpene Composition and Antioxidant Activity of Four Ganoderma Species: A Chemometric Analysis. Chem. Biodivers. 2025, 22, e202500206. [Google Scholar] [CrossRef] [Scilit]
  197. Thakkar, S.; Anklam, E.; Xu, A.; Ulberth, F.; Li, J.; Li, B.; Hugas, M.; Sarma, N.; Crerar, S.; Swift, S.; et al. Regulatory landscape of dietary supplements and herbal medicines from a global perspective. Regul. Toxicol. Pharmacol. 2020, 114, 104647. [Google Scholar] [CrossRef] [Scilit]
  198. U.S FDA. 2016. Available online: https://www.fda.gov/regulatory-information/search-fda-guidance-documents/botanical-drug-development-guidance-industry (accessed on 7 February 2026).
  199. Calin, A.; Burlec, A.F.; Mircea, C.; Macovei, I.; Hancianu, M.; Corciova, A. Evolution and Comparative Analysis of Clinical Trials on Psilocybin in the Treatment of Psychopathologies: Trends in the EU and the US. J. Clin. Med. 2025, 14, 6613. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Schematic representation of the derivation of raw mushroom material with pharmaceutical-relevant bioactive profile (authors’ own creation).
Processes 14 00795 g001
Figure 2. Conceptual illustration of conventional and non-conventional extraction methods applied to edible mushrooms for the recovery of pharmaceutical-relevant bioactive compounds (authors’ own creation).
Processes 14 00795 g002
Figure 3. Isolation and Purification Workflow for Bioactive Compounds from Edible Mushrooms (Author’s own creation).
Processes 14 00795 g003
Table 1. Comparative overview of conventional and advanced extraction techniques for mushroom bioactive compounds.
Extraction MethodTypical Extraction DurationOperating Temperature (°C)Volume of Organic Solvent UsedExtraction EfficiencyKey AdvantagesMajor Limitations
Hot-water extraction1.5–5 h50–80NoneModerateEconomical; simple operation; no need for sophisticated equipmentHigh risk of degradation of thermo-sensitive compounds
Hydro-alcoholic extraction1–24 h25–60LargeVariableEfficient for extracting both polar and moderately non-polar compoundsHigh solvent consumption; reliance on costly organic solvents
Enzyme-assisted extractionModerate<50ModerateHighMild operating conditions; environmentally friendly; enhances selectivity and impurity removalRequires specialized expertise; efficiency depends on enzyme stability and digestion time
Pressurized liquid/subcritical water extractionShort>100SmallHighAutomated operation reduces human error; improves extraction efficiency and analyte stabilityThermal degradation of heat-sensitive compounds; co-extraction of impurities under high pressure; expensive specialized equipment
Supercritical fluid extractionModerateAbove critical pointNoneVery HighGreen technology using CO2; highly efficient for non-polar compoundsHigh operational cost; technical complexity; safety concerns due to high pressure
Ultrasonic-assisted extractionShort40–60ModerateHighLow energy consumption; compatible with various solvents; enhances mass transferEfficiency influenced by ultrasonic attenuation; energy loss in bath systems
Microwave-assisted extractionShortRoom temperatureNone or moderateHighRapid heating; reduced solvent use; high selectivity; minimizes thermal degradation when low-polarity solvents are usedRisk of mechanical or thermal damage to bioactive compounds; high equipment cost; requires pressure-resistant and airtight systems
Sources: Refs. [12,18,99].
Table 2. Application of conventional solvent-based methods for extraction of bioactive compounds from edible mushrooms.
Mushroom Material (Pre-Treatment)Extraction SolventExtraction Conditions (Time/Temperature)Solvent-to-Solid RatioTarget Bioactive Compound(s)Extraction YieldReference
Lentinula edodes (freeze-dried and ground into 1.75, 3.35, and 4.75 mm)Hot waterWater bath; 5 h/45 °C2.5% w/vTotal phenolics11.29 mg GAE/g[98]
EthanolIncubated at 90 °C for 1 h40% v/v3.68 mg GAE/g
Pleurotus sajor-caju—air dried and knife-milledEthanol or hexaneSolvent recycling in a Soxhlet apparatus for 6 h at solvent boiling temperature1:30 g/mLTotal phenolics15.6% (ethanol); 1.2% (hexane)[103]
C. cibarius, Morchella spp., B. edulis—freeze-dried
Agaricus bisporus, L. deliciosus, P. ostreatus, L. edodes—tray dried
Hericium erinaceus, and G. lucidum—obtained dried
Methanol (M), water (W), and W/M (50:50 v/v)Extracted with a mechanical shaker at 4 °C for 10 h1:10 g/mLTotal phenolics0.65 to 17.11 mg GAE/g d.w., depending on the solvent type and species[104]
P. ostreatusWaterBoiled at 100 °C over a period of 3 h1:20 w/vPolysaccharides6.21% yield[105]
Panus conchatus (fermentation broth)WaterBathed at 95 °
C for 1 h
1:1 v/vErgothioneineVaried depending on the carbon and nitrogen sources used for cultivation[106]
Freeze-dried forms of Aleuria aurantia, Phallus hadriani, and Panus conchatus ground into powder using an electric grinderEthanolHeated on a heating bowl at boiling point for 10 min1000 g of powdered mushroom fruiting body was poured into 10 mL of absolute ethanolPolyphenols0.617–1.501 mg GAE/100 g[107]
Lycoperdon saccatum, P. ostreatus, Craterellus cornucopioides, Russula cyanoxantha and C. cibarius—air dried and ground in a blender into 0.132 mm, 0.277 mm, 0.433 mm, 0.294 mm and 0.347 mm, respectivelyHexaneUsing a Soxhlet apparatus with an attached reflux condenser for 8 h at 40 °C3.33% w/vLipids (fatty acids and sterols)0.83–3.38%[108]
Laetiporus sulphureus—lyophilised and reduced to a fine dried powder (20 mesh)Methanol, ethanol and waterStirred with solvent at 30 °C for 24 h10% w/vTotal phenolics230 (methanol), 65.7 (ethanol), and 47.4 (water) μg GAEs per mg[109]
Naturally dried T. versicolor ground into fine powder (40 mesh) using a laboratory grinderWater4 h at 95 ± 5 °C1:10 w/vTotal phenolics433.98 mg GAE/100 g[110]
H. erinaceusEthanolSoxhlet extraction under optimum conditions (61 °C temperature, 7 h 50 min, and 2 mg/mL)NAPhenolic compounds59.75 mg/g[111]
Hypsizygus marmoreus—freeze-dried and ground into powderWaterMechanically stirred at 10 °C for 6 h10% w/vPolysaccharidesNA[112]
Dried and powdered P. ostreatus, G. lucidum, Fomes fomentarius, Porodaedalea pini, Fuscoporia torulosa, and Phellinus igniariusEthanol and water in a sequential order80% ethanol at room temperature for 24 h; followed by water at 80 °C NAPolysaccharidesNA[113]
Lentinus squarrosulus, Auricularia auricular-judae, Mycetinis copelandii, Baeospora myosura, P. ostreatus, and Volvariella volvacea—air-dried and grind into powder with an electronic blenderMethanolHeated at 30–40 °C in a Rotary Evaporator10% w/vLipidsNA[114]
Agaricus campestris, Macrolepiota procera, C. cibarius,
Russula vesca, Russula alutacea, B. edulis, P. ostreatus, and A. bisporus
Water and 50% water–ethanolStirred at room temperature for 4 h4% w/vPolyphenols (flavonoids)7.61–31.78 mg GAE/g d.w. for water extract
9.28–69.65 mg GAE/g d.w. for hydro-ethanol extract
[115]
Lyophilized basidiocarps of P. ostreatusCold and hot waterCold distilled water (25 °C with continuous magnetic stirring) and boiling water (100
°C under reflux) for 7 h per extraction
16.67% w/vPolysaccharides3.40% (hot water)–6.14% (cold water) w/w[116]
Fruiting bodies of Lentinus velutinus—dried in hot air oven and blended into fine particlesWater and EthanolMushroom biomass was boiled three times with 20 volumes of water for 3 h each, followed by 80% ethanol at 4 °CNAPolysaccharides3.99% yield[117]
B. edulis and C. cibariusAcidic water-10% (v/v) acetic acid solution; a mixture of ethanol, water and acetic acid; hexane; and diethyl etherOrbital shaking at room temperature for 24 h3.33% w/vPolyphenolsB. edulis: 0.48–3.73 mg GAE/g
C. cibarius: 0.29–0.79 mg GAE/g
[118]
Ganoderma neo-japonicumWater and ethanolBoiling for 4 hNAPolysaccharidesNA[119]
Powdered Pleurotus flabellatusMethanolUsing a Soxhlet extractor for 4–5 h at a temperature below the solvent boiling point10% w/vMultiple class of bioactive compoundsNA[120]
Dried fruiting bodies of Paxillus involutusEthyl acetateExtracted at room temperature for 3 days16.5% w/vPhenolics (novel 2,5-diarylcyclopentenone derivatives)883 g crude extracts[121]
L. edodes, V. volvacea, Pleurotus eous, P. sajor-caju and A. auricula (freeze-dried and finely milled)WaterBoiled for 30 min2% w/vTotal phenolics2.90–36.19 mg GAE/g dw[122]
50% (v/v) ethanolRoom temperature for 24 h10% w/v2.75–27.89 mg GAE/g dw
Diethyl etherRoom temperature for 24 h10% w/v1.99–10.46 mg GAE/g dw
Inonotus obliquus (pulverized using a blender)Hot waterRefluxed for 2 h in a water bath at 100 °C2.5% w/vTotal glucans, total triterpenoids3.81% w/w (total glucan)
8.90 mg UAEq/g (total triterpenoids)
[123]
A. auricula judae, Microporus xanthopus, Termitomyces umkowaani, Trametes elegans, and T. versicolor—oven dried and powdered99.8% Chloroform, 70% ethanol, and hot waterMushroom material was separately combined with each solvent in an Erlenmeyer flask at 25 °C and shaken in an incubator for 72 h10% w/vMultiple compounds, including carboxylic acids, phenols, fatty acids, isoprenoid lipids, and steroidsVaried depending on the species and bioactive compound[124]
Dictyophora indusiata—air dried and fully ground into powder by a high-speed pulverizerHot waterWater bath at 88 °C for 2.5 h1:40 g/mLPolysaccharidesLowest yield compared to other non-conventional extraction methods (UAE, MAE) [125]
L. edodes—flash-frozen and ground into fine particles using a cryogenic grinderEthyl acetate, ethanol, ultrapure water, cyclohexane, and dimethyl sulfoxide (DMSO)24 h at 4 °C1:10 g/mL Secondary metabolites, including indole-3-lactic acidWater and cyclohexane extracts had the highest number of total compounds, followed by DMSO, ethanol, and ethyl acetate extracts[126]
NA—not reported in the cited study; UAEq—ursolic acid equivalent; GAE—gallic acid equivalent.
Table 4. Structural elucidation and analytical characterization of bioactive compounds isolated from edible mushrooms.
Edible Mushroom SpeciesIdentified Bioactive Compound(s)Chemical Class of CompoundMolecular Weight/FormulaAnalytical Techniques EmployedMonosaccharide/Amino Acid CompositionKey Structural FeaturesReported BioactivityReference
D. indusiataNAPolysaccharides1534–24,110 kDaFT-IR, NMR (1H), HPSEC-MALLSFuc, Ara, Gal, Glc, Xyl, Man, Fru, GlcANMR analysis indicated strong interactions between bound water molecules and polar functional groups on the polysaccharide surface, suggesting a highly hydrated macromolecular structureAntioxidant activity[125]
P. involutus2,5-diarylcyclopentenone derivatives (involutenones A–H)Phenolic compoundsC18H14O6 (A), C18H14O7 (B), C27H24N2O7 (C), C21H17NO5 (D), C22H19NO7 (E), C19H16O8 (F), C18H14O7 (G), C18H16O7 (H)NMR (1H and 13C), HRESI-MSNAAbsolute configurations of selected involutenones were established through comparison of experimental and calculated electronic circular dichroism (ECD) spectraAntioxidant activities[121]
B. edulisKBMPHF 1-4PeptidesKBMPHF1 (>10 kDa), KBMPHF2 (3–10 kDa), KBMPHF3 (1–3 kDa), and
KBMPHF4 (<1 kDa)
LC-MS/MSAlanine, arginine, asparagine, aspartic acid, cysteine, glutamic acid, glutamine, glycine, histidine, isoleucine, leucine, lysine, methionine, phenylalanine, proline, serine, threonine, tryptophan, tyrosine and valineACE-inhibitory activity of low-molecular-weight peptide fractions was associated with hydrogen bonding interactions and the presence of hydrophobic cavitiesAntioxidant activity, ACE inhibition[168]
P. ostreatus and G. lucidumNAPolysaccharidesNANMR (1H and HSQC) and GC–MSGlc (86%), Man (4.9–9.4%) and Gal (1.1–3.5%)NMR (HSQC) analyses revealed that all extracts of both mushrooms contained mainly α- and β-glucans and heteropolysaccharides with branched and linear (1→3) and (1→6) linkagesNA[155]
H. marmoreusFucomannogalactan (FMG-Hm)Hetero-polysaccharide17.1 kDaHPSEC-RI, GC–MS, NMR (1H, HSQC-edit, HSQC-TOCSY, HSQC-NOESY)Fuc, Man, and Gal (1:1.08:3.17)Structural analyses confirmed a branched fucomannogalactan composed of an α-(1→6)-linked galactopyranosyl backbone partially substituted at O-2 with terminal α-L-fucopyranose and β-D-mannopyranose residuesAntimelanoma property[112]
A. melleaAMPPolysaccharidesNAFT-IR, HPLCMan, Rha, Glc, Gal, and Fuc, with varying ratios depending on the extraction methodFT-IR revealed presence of O-H bending vibration, C-H stretching vibration, C = O stretching vibration, and C-H variable angle vibration, as well as presence of pyranoseAntidiabetic activity[141]
P. eryngiiPEP-0.1-1, PEP-0-1 and PEP-0-2Polysaccharides3235 kDa, 2041 kDa, and 23.933 kDa for PEP-0.1-1, PEP-0-1, and PEP-0-2 respectivelyUV-vis, FT-IR, HPLC, NMR (1H, 13C NMR, COSY, HSQC, HMBC, NOESY)PEP-0.1-1 contained Gal and Glc (6.63:93.37);
PEP-0-1 contained Fru, Gal, Glc, Xyl, Man, and Fru (0.14:0.73:94.2:0.61:2.79:1.53);
PEP-0-2 contained Fru, Gal, Glc, Xyl and Man (0.64:16.62:68.56:0.51:13.67)
FT-IR and multidimensional NMR analyses revealed pyranose ring structures with C–O–C glycosidic linkages; PEP-0.1-1 exhibited a linear (1→4)-linked glucopyranosyl backbone, whereas PEP-0-1 and PEP-0-2 displayed branched (1→4)-Glcp and (1→6)-Galp linkagesAnti-inflammatory activity[142]
PEPProtein40 kDaMALDI-TOF-MSNAPEP shared partial amino acid sequence homology with the known protein Pleery1 (48 kDa); however, its distinct molecular weight led the authors to classify PEP as a novel protein isolated from P. eryngiiAnti-inflammatory activity[183]
P. baumiiPBMP1Polysaccharide2.95 × 103 kDaHPLC, GC-MS, FT-IR, NMR (1H, 13C)Fuc (1%), Glc (24.54%), and Gal (0.29%)FT-IR and NMR analysis confirmed that PBMP1 is a hetero-polysaccharide with an α-glycosidic linkage and highly branched 1,3,4-Glc and 1,4,6-Glc branches with Fuc as the non-reducing terminusNA[182]
P. ostreatusNAPolysaccharidesNAFT-IR, XRD, NMR (1H)NAThe anomeric bonds identified using FT-IR and NMR analyses indicate that the extracts are a mixture of heteropolysaccharides, β-glucans, α-glucans, and oligosaccharideAntioxidant activity[105]
GC-MS, FT-IR, NMR (1H, 1H COSY and 1H, 13C HMQC)Glc, Fuc, Rha, Gal, Xyl, Man, AraCold- and hot-water-soluble fractions contained a branched partially methoxylated mannogalactan and slightly branched (1→6)-β
-D-glucan, respectively; the DMSO-insoluble polysaccharide was identified as linear (1→3)-α-D-glucan, while the DMSO-soluble one was a branched
(1→3)(1→6)-
β-D-glucan
NA[116]
A. campestris, M. procera, C. cibarius,
R. vesca, R. alutace, B. edulis, P. ostreatus, and A. bisporus
NAPhenolic compoundsNAFT-IRNASpectral data for extracts confirmed the presence of bioactive functional groups including, –OH, >NH, –CHO, –COOH, and –COOR; all extracts exhibited the presence of a broad peak for hydrogen bonded –OH stretchingAntioxidant activity[115]
C. sinensisCSF1, CSF2 and CSF3Nucleosides, polyphenolsNAHPTLC, GC-MSNAHPTLC confirmed the presence of flavonoids (ascorbic acid, gallic acid and quercetin) and nucleobases while GC-MS analysis revealed VOCs (e.g., α-linoleic acid, 9,12-octadecadienoic acid (Z,Z)-, trimethylsilylester)Antibacterial and hypoxia-protective activities[152]
L. edodesLE331Indole derivativesC11H11NO3HPLC, LC-MS, NMR (1H and 13C)NAIdentification of the most cytotoxic isolate by LC-MS and 1D NMR revealed it to be 2-
hydroxy-3-(1H-indol-3-yl) propanoic acid, also known as
indole-3-lactic acid (ILA)
Anticancer activity[126]
T. lobayenseTLH-3 and TLH-3′Polysaccharides4.24 kDa and 4.23 kDa for TLH-3 and TLH-3′, respectivelyFT-IR, HPLCRha, Man, GlcA, GalA, Glc, Gal, AraMolecular weights, FT-IR, and monosaccharide composition analysis concludes that TLH-3 and TLH-3 are the same polysaccharideAntioxidant activity[177]
R. botrytisRBUPProtein18.5 kDaESI-MS/MSNAESI–MS/MS sequencing revealed that RBUP shares 69% amino acid sequence similarity with ubiquitin from Coprinellus congregatusHemagglutinating and antitumor activities[185]
A. cinnamomea, C. versicolor, G. frondosa, G. lucidum, and P. LinteusNAPolysaccharides 10.2–722.7 kDaHPSEC, FT-IRFuc, Gal, Glc, Man, Rha, Rib, Xyl, GalA, GlcAAll mushroom extracts contained (1→3;1→6)-β-D-glucans in varying proportions; the degree of branching of (1→3;1→6)-β-D-glucans in all polysaccharides ranged from 0.21 to 0.26; the authors similarly reported the existence of triple-helix structures in the samplesImmunomodulatory activity[171]
P. pulmonariusNALipidsNAGC-FID, GC-MS, HPLCNAGC analysis detected 136 chemical constituents, with 9-oxononanoic acid, linoleic acid, oleic acid, stearic acid, and ethyl octadecanoate being the most abundant in all of the extracts; HPLC also confirmed the presence of ergosterolAntioxidant activity[153]
L. velutinusLVPPolysaccharide336 kDaFT-IR, SEC, TLCOnly glucoseFT-IR revealed that LVP is a polysaccharide with sugar ring structuresAnticancer and antioxidant activities[117]
P. sajor-cajuNAPhenolic compounds and lipidsNAGC-MS, LC-ESI-MS/MSNAGC-MS and LC-ESI-MS/MS analyses identified compounds belonging to phenols and lipids, with linoleic, chlorogenic and vanillic acids being the major compoundsAntioxidant and antimicrobial activities[103]
NA—not reported in the cited study; HRESI-MS—High-Resolution Electrospray Ionization Mass Spectrometry; HPSEC-MALLS—High-Performance Size-Exclusion Chromatography coupled with Multi-Angle Laser Light Scattering; HSQC—Heteronuclear Single Quantum Coherence; RI—refractive index detector; TOCSY—Total Correlation Spectroscopy; NOESY—Nuclear Overhauser Effect Spectroscopy; UV-vis—ultraviolet-visible spectroscopy; HMBC—heteronuclear multiple bond correlation; HPTLC—high-performance thin layer chromatography; ESI–MS/MS—electrospray ionization-tandem mass spectrometry; GC-FID—gas chromatography flame ionization detector; kDa—Kilodalton. Monosaccharide notation: Glucose → Glc; Galactose → Gal; Mannose → Man; Fucose → Fuc; Rhamnose → Rha; Xylose → Xyl; Arabinose → Ara; Fructose → Fru; Ribose → Rib; Glucuronic acid → GlcA; Galacturonic acid → GalA.
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.