2. Normalized Equations and Single Coupling Parameter
The classical nonlinear LV model is based on four time-independent, positive, and constant rates with two representing species self-interaction, i.e., natural exponential growth rate and decay rate per individual of the respective prey and predator populations, and two other rates characterizing inter-species interaction.
Without any loss of generality, the standard LV system of two coupled 1st-order ordinary differential equations (ODEs) can be simplified by simultaneously scaling the predator and prey populations together with time
through a dimensionless time factor
. The system is shown to only depend on a positive coupling parameter
, ratio of the respective growth and decay rates of each species taken separately [
7], defined as
The respective instantaneous prey and predator populations, labeled
u and
v, both ⩾0, are assumed to be continuous functions of time (
). A normalized form of the LV system is obtained as a set of two coupled 1st-order nonlinear ODEs solely depending on this single coupling ratio
. The time evolution of the two species is modeled as a system of two coupled autonomous nonlinear ODEs where the “dot” on
and
indicates a derivative with respect to the dimensionless time
tNumerous solutions of system (2) have been developed, including trigonometric series [
8], mathematical transformations [
9], Taylor series expansions [
10], perturbation techniques [
11], Lambert W-functions [
12], and numeric-analytic techniques [
13].
In the sudden absence of coupling between species, the prey population grows at an exponential rate , while predators similarly decay at an inverse rate from their respective positive initial values. Remarkably, the normalized ODE system (2) is invariant in the transformation together with . This fundamental property, subsequently referred to as “ invariance”, is extensively used throughout to considerably simplify the LV problem analysis.
Since the original publications [
1,
2], the non-trivial system (2) has been known to possess a dynamical invariant or “constant of motion
K”, expressed here in
-
invariant form:
The objective of this research is to formulate the LV problem in a simple form while attempting to uncouple the basic ODE system: the introduction of new “hybrid species” enables uncoupling the LV system into 2 ODEs with one being linear.
In the following sections, a particular functional transformation combined with a suitable linear change of variables defines a novel λ-invariant Hamiltonian based on these hybrid variables, thereby reducing the system (2) to a new set of two 1st-order ODEs with one being linear. As a result, an exact analytic solution is derived for one hybrid function in terms of a simple quadrature. An original approximate method uncouples the system, yielding approximate analytic quadrature solutions of the LV problem. The LV oscillation period as a function of the coupling parameter and the system’s energy h is further presented. At high energies, closed-form asymptotic solutions are derived.
In the special case of , the LV system completely uncouples into two 1st-order ODEs, with one being linear and the other being autonomous. An exact analytic solution is derived for each hybrid function separately in terms of a single quadrature expressed in terms of the Lambert W function. An exact analytic solution of the LV system for each individual prey and predator species and is also derived. The exact population oscillation period is further presented in terms of a dimensionless energy function.
The
case represents a physically more realistic case in ecology, whereas the
case can also be interpreted as a (rare) competitive case in which the prey is another predator: it corresponds to the ecological condition
, i.e., equal intrinsic growth and decay rates of prey and predator. While non-generic, it is more than a mathematical idealization since it is a special ecologic condition that provides the one case where the uncoupling (23) is exact, serving as a benchmark for the accuracy of the general case
approximation. Lastly, it should be mentioned that an exact solution of the LV system has previously been derived [
14] in the case when
: this non-ecologic condition precludes population oscillation.
3. Solutions with Hybrid Predator–Prey Species
A logarithmic functional transformation originally introduced by Kerner [
15] proposes to modify the coupling between the respective species through a change of variables according to
The LV system (2) for the respective “logarithmic” prey-like and predator-like species
and
becomes
Similar to (2) this
-
invariant system (
5) admits a primary conservation integral
H expressed as the linear combination of two positive convex functions
As already established [
16,
17],
is the time-independent Hamiltonian of the LV system since (
5) satisfies Hamilton’s equations with
x as the coordinate conjugate to the canonical momentum
y. Equation (
6) expresses the conservative coupling between species
and
. It is further rendered
-
invariant by introducing a scaled Hamiltonian
with total constant positive energy simply labeled
h according to
A
-
invariant linear 1st-order ODE between the species
and
is introduced by further combining the system (
5) with (
6) and (
7)
This linear differential Equation (
8) suggests introducing a
final λ-invariant linear transformation of the set {
x(t),
y(t)} to a new set {
ξ(t),
η(t)} representing a symbiotic association between predator and prey species in which each hybrid function of the new set of canonical Hamiltonian variables {
ξ(t),
η(t)} is a
linear combination of the original predator and prey populations. This is the unique combination of
x and
y that converts the linear ODE (
8) into the canonical form
(see (17a)) by requiring the coefficient structure of (
8) to match a momentum or coordinate pair of Hamilton equations,
The original Hamiltonian (
6) together with Equation (9) and the linear transformation (
7) then becomes
Here
is a new Hamiltonian for the coordinate
and conjugate momentum
. Notice that, for small amplitudes,
is a harmonic oscillator Hamiltonian. Upon further introducing the following
-
invariant G function
the conservation relationship (
10) between the conjugate functions
η(t) and
ξ(t) is recast into a compact form that naturally separates the variables,
In the following, a useful compact auxiliary function
U(ξ) appearing throughout is defined as
Even though still nonlinear, the conservation relationship (
12) partially uncouples the
ξ(t)-function from the
η(t)-function, resulting in three essential
G-function properties:
From (
12), the
function thus oscillates between the respective negative and positive roots
and
, turning points of the equation
; i.e.,
. These are naturally expressed in exact closed form in terms of the Lambert W function [
18] as
where the index
k refers to the respective
and
branches of the Lambert W function since
. The roots are displayed in Table 2 in
Section 4 for several increasing values of
h.
In the
plane, (
12) represents a symmetric closed-orbit mapping around the fixed point
in closed form. On the
horizontal axis this orbit is bounded by the limits
and
, and, since
U(ξ) admits a maximum
located at
, it is also bounded by the two respective positive and negative root solutions of the equation
. For any given energy
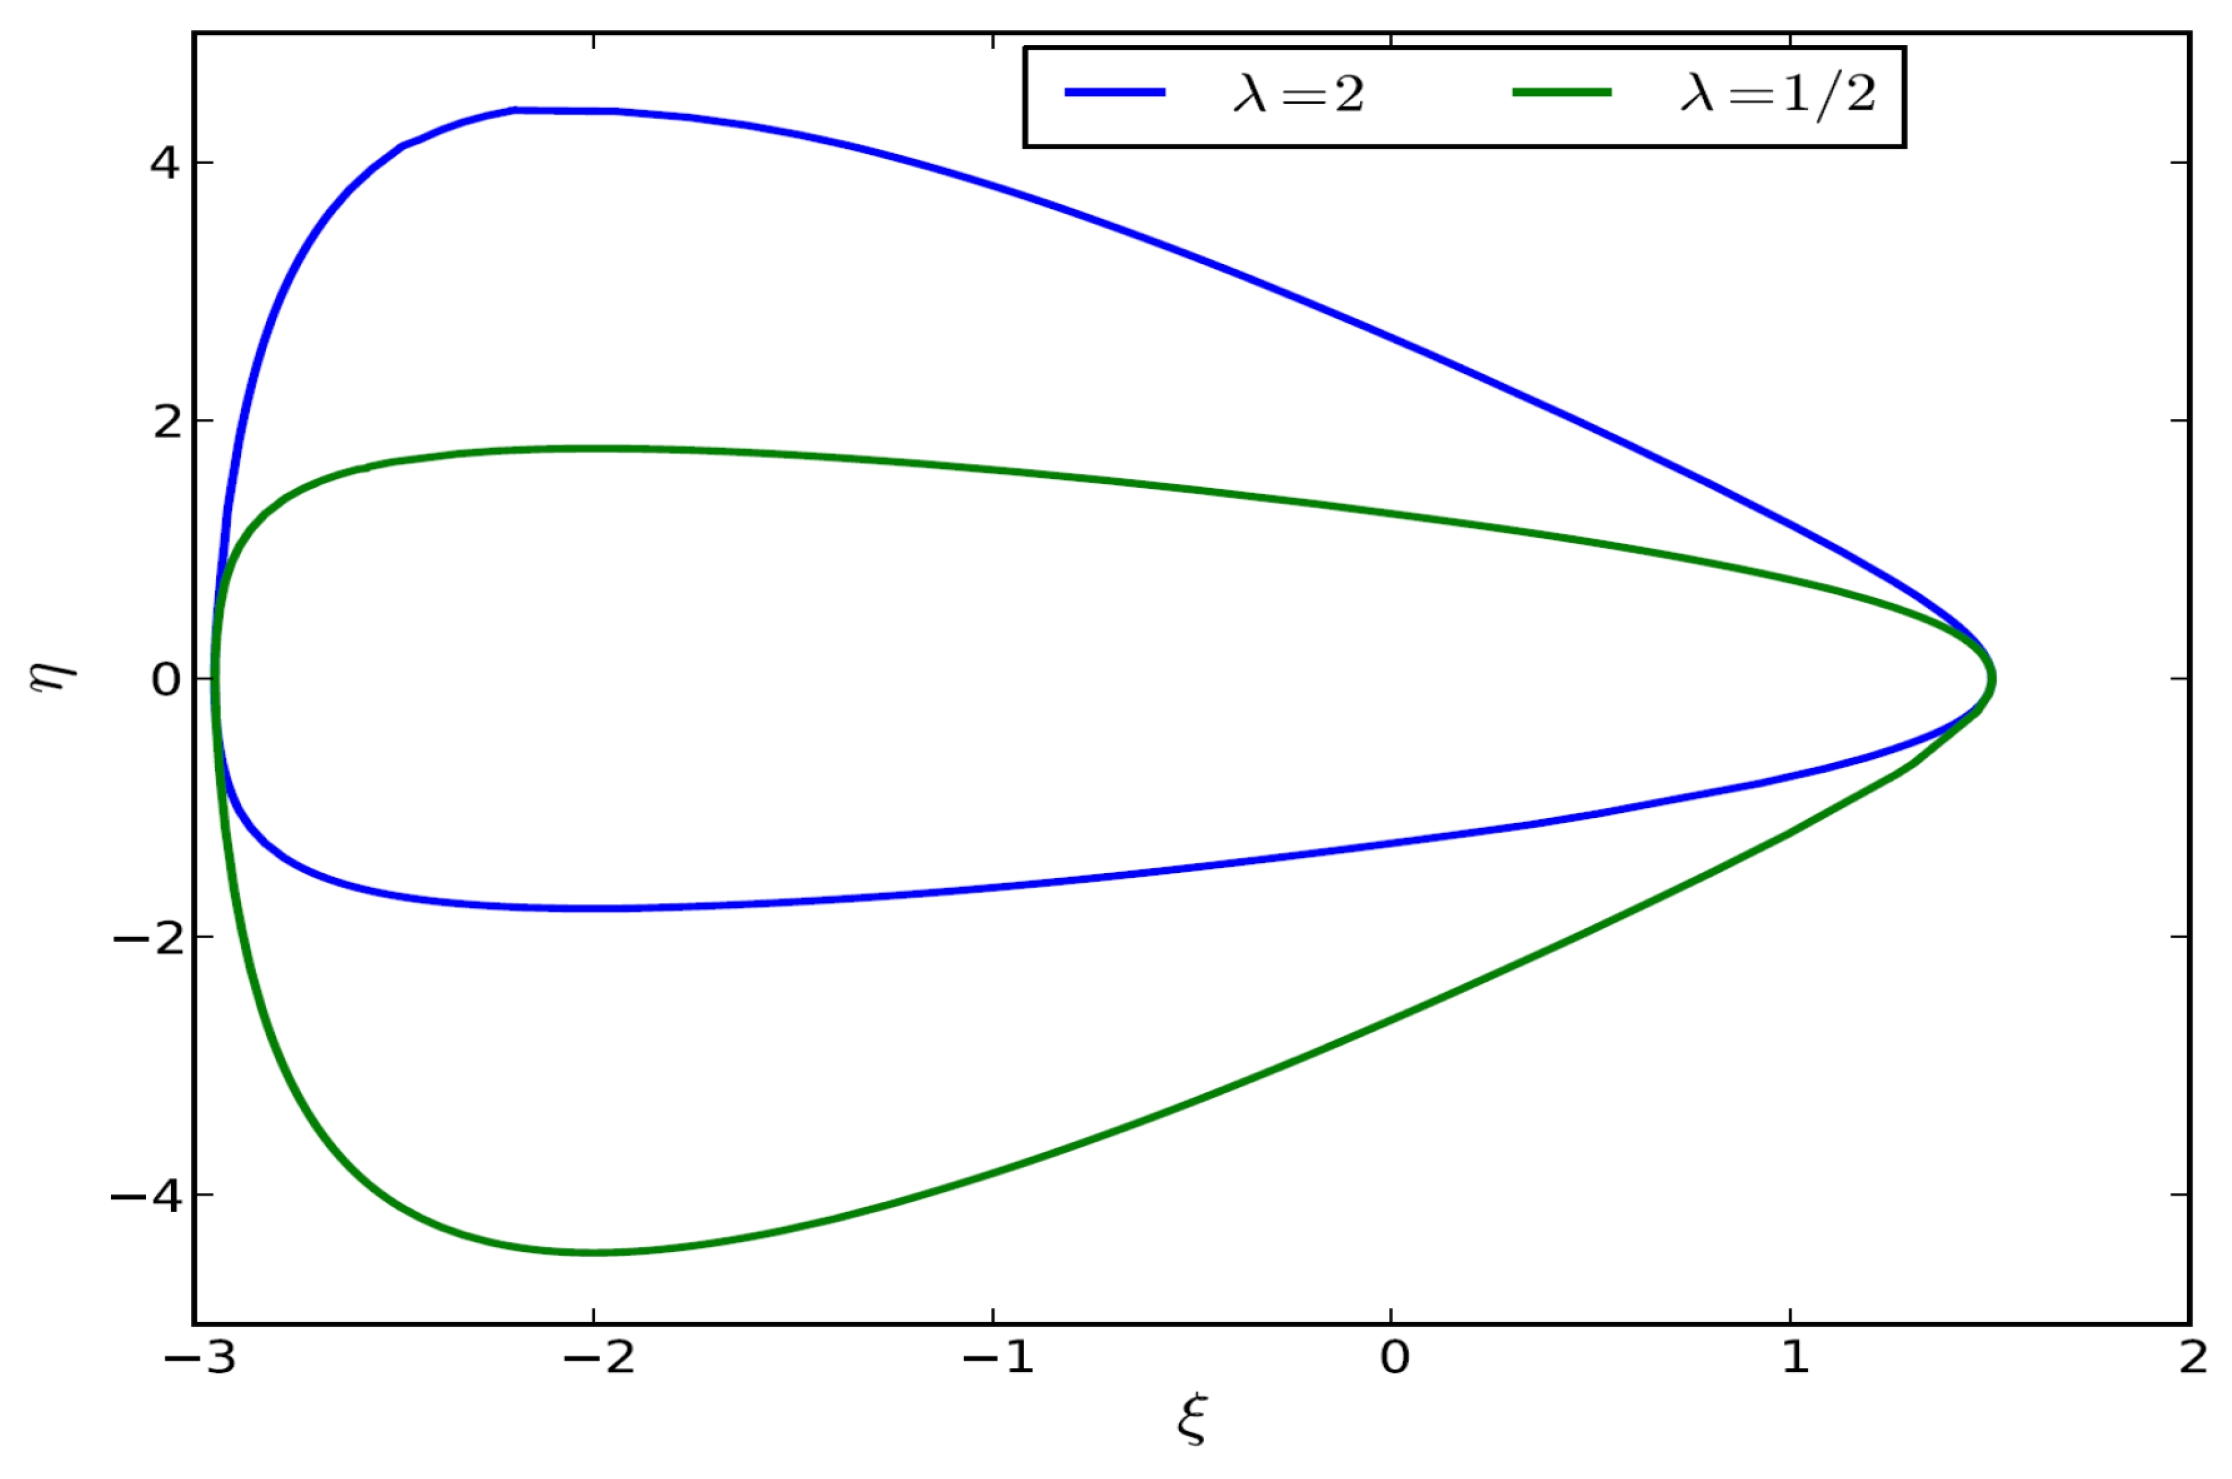
h this orbit consists of two respective branches,
and
, associated with the decay and growth of
, the switch occurring at the tuning points, as displayed in
Figure 1, where the respective values chosen are
and coupling ratios
and
. Per (
12), the respective branches associated with the
and
mappings are readily observed to be mirror images of each other with respect to the
axis.
Except when
, algebraic solutions of (
12) may generally not be obtained directly. However, for any value
, the two roots
of (
12) may numerically be obtained through a standard Newton–Raphson algorithm: each root admits lower and upper bounds for any value of
U(ξ), thereby ensuring algorithm convergence [
7].
Lastly, upon inserting the linear transformation (9) into the modified LV system (
5), or equivalently using the standard Hamilton equations with (
10), a new
semilinear system of coupled 1st-order ODEs is obtained:
The solution of the system (17), in which
is the derivative
, represents the time evolution of the hybrid functions
and
. However, due to the linear transformation (9), the first coupled equation (17a) becomes
linear since it directly expresses ODE (
8). Remarkably, up to the constant energy
h, the time derivative of the function
is directly equal to the instantaneous value of
, thereby simplifying the solution of (17). The exact solution of the LV problem is then derived by integration of the linear ODE (17a) as a
simple quadrature for
, with time as a function of
. Upon using the initial conditions
and
when
, the exact LV solution corresponding to the respective negative and positive branches
and
becomes
This quadrature does not diverge at
since the numerator of the differential
contains
. Upon using the same initial conditions for
and
, (
18) is expressed in terms of the continuous function
itself through a
standard integration by parts in which the singularity at
is further eliminated by adding and subtracting the expression
in the integral. The final exact regular solution of the LV problem for any value of the coupling ratio
and any value of the orbital energy
h is thus expressed as a
simple quadrature over each of the two branches
that are solutions of (
14) (Consider
; since
vanishes at
, taking the derivatives of both sides implies
(obvious from the graph of
Figure 1). Upon calling
the numerator of the integral in (
19) so that
and
, then
. In the limit
, by l’Hopital rule, the 1st term in (
19) vanishes since it is the definition of the derivative
, while the 2nd term is manifestly finite since
never coincides with the turning points. As
the integrand of the (
19) integral equals
, which is finite. Therefore (
19) is convergent at
.)
This solution for is further analyzed below. Even though the oscillation of is not explicitly expressed as a function of time t, the function t(ξ) being monotonic and continuous on each respective integration interval defined above, its inverse function , defined by , exists and is unique, monotonic, and continuous on each interval.
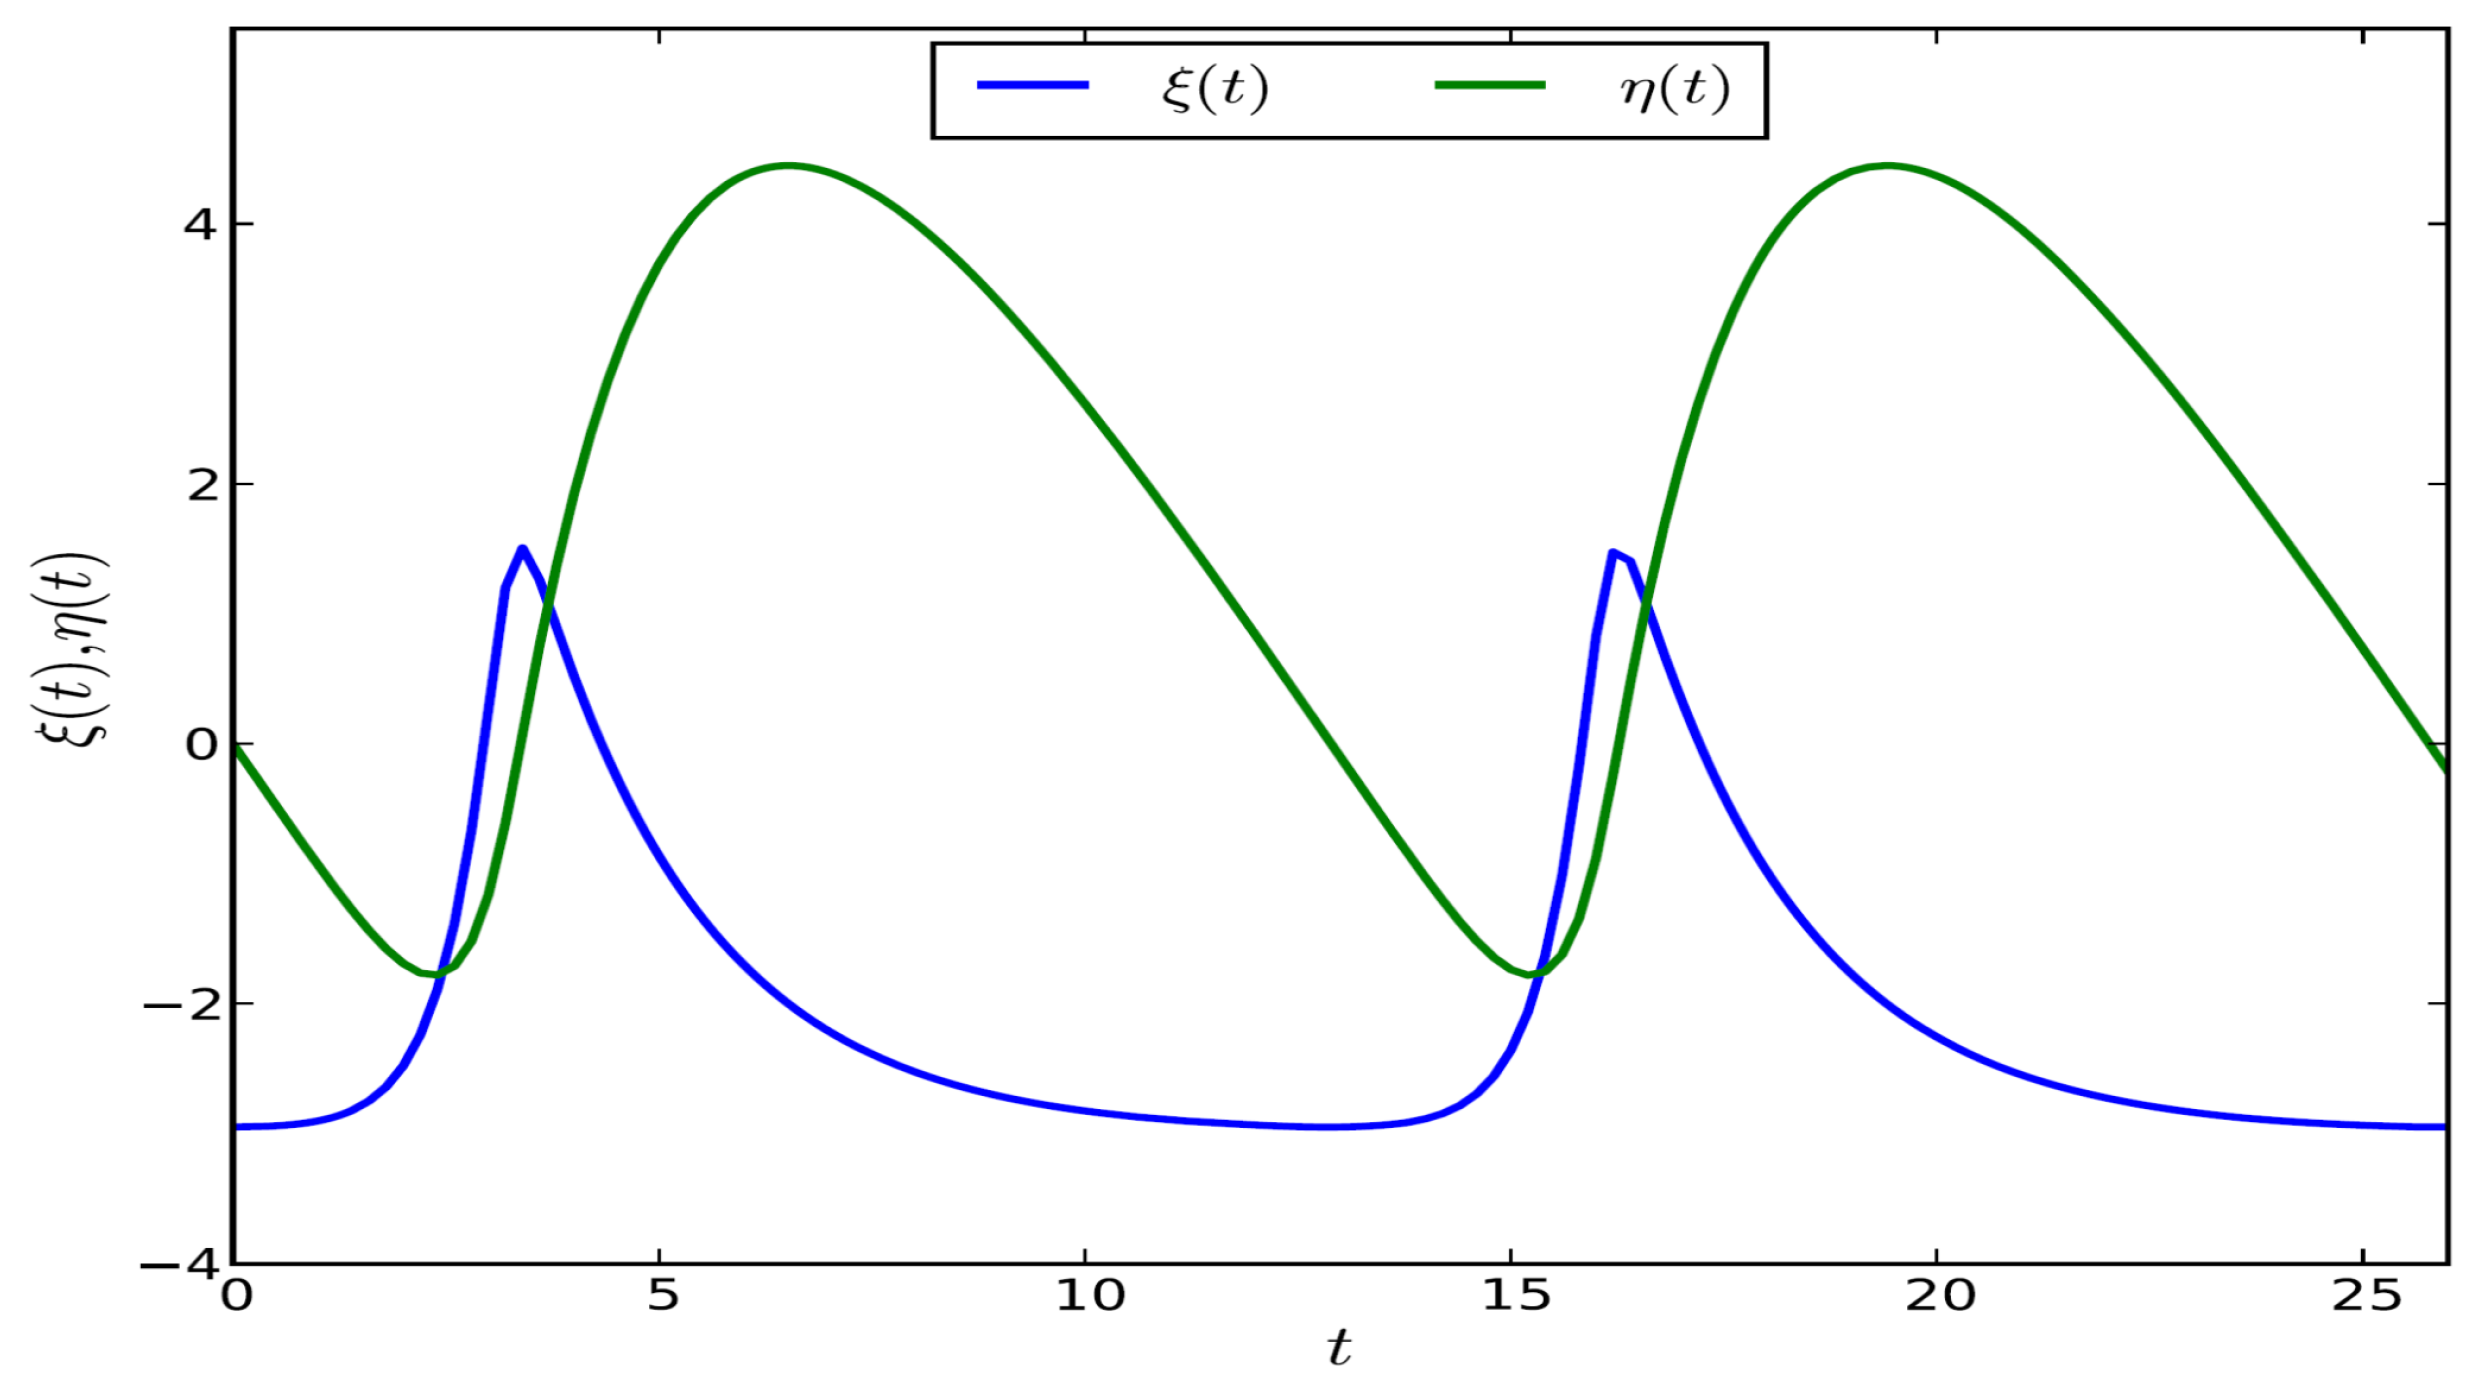
Numerical solutions for
and
are also obtained by integrating (17) using a standard fourth-order Runge–Kutta (RK4) method as presented in
Figure 2 for values of
h and
that are identical to those of
Figure 1, together with initial conditions
and
, defined above. The function
is observed to principally depend on two time constants: a quasi-exponential increase at a rate of order
followed by an exponential decrease at a rate
. Its amplitude
only depends on the system’s energy. As expected from
invariance, the two functions
respectively corresponding to the coupling ratio
and its inverse
are mirrors of each other; so are the functions
but with the change
.
It may generally not be possible to algebraically solve (
12) for
for insertion into the integral solution (
19). A strategy consists of eliminating the
dependence in (17b) and seeking an ODE for
only. An approximate relationship explicitly relating
to its derivative
and expressing the latter as an analytic function of
only through (
12) is derived below.
3.1. Case
This particular case is exactly solved since an explicit relationship exists between
and
, namely (omitting the index for simplicity)
The
G function (
11) reduces to the hyperbolic cosine function; the conservation Equation (
12) becomes a closed-form expression,
The resulting
–
closed-orbit mapping is symmetric. On the
axis, for any value of the energy
h, the closed-form mapping is bounded by
and
. The two symmetric branches
around the fixed point
are explicitly expressed as
The negative branch is associated with the growth phase of , whereas is associated with the decay. The orbit is bounded by the turning points and on the horizontal axis, and, since admits an extremum located at , it is also bounded on the vertical axis by the two respective roots of the equation .
Lastly, inserting (
22) into (17) yields a new
system of two 1st-order ODEs for each hybrid function taken separately, with the evolution of
represented by a 1st-order nonlinear
autonomous ODE,
The solution of system (23) represents the periodic time evolution of both functions and . Remarkably, in this case, the LV problem solution is simplified since a solution of the autonomous Equation (23b) only is required.
The linear Equation (
23a) is directly solved by inserting
from (
22) into the solution (
19). Together with
defined in (
13), the exact analytic solution on the interval
is thus expressed as a simple
quadrature in terms of elementary functions
By applying l’Hôpital’s rule, it is readily verified that the integrand in (
24) is regular at
. For a given energy
h, solutions for
can be obtained by numerical integration of (
24). The complete solution of the LV problem for
is finalized for
by inserting
, derived above, into (
22).
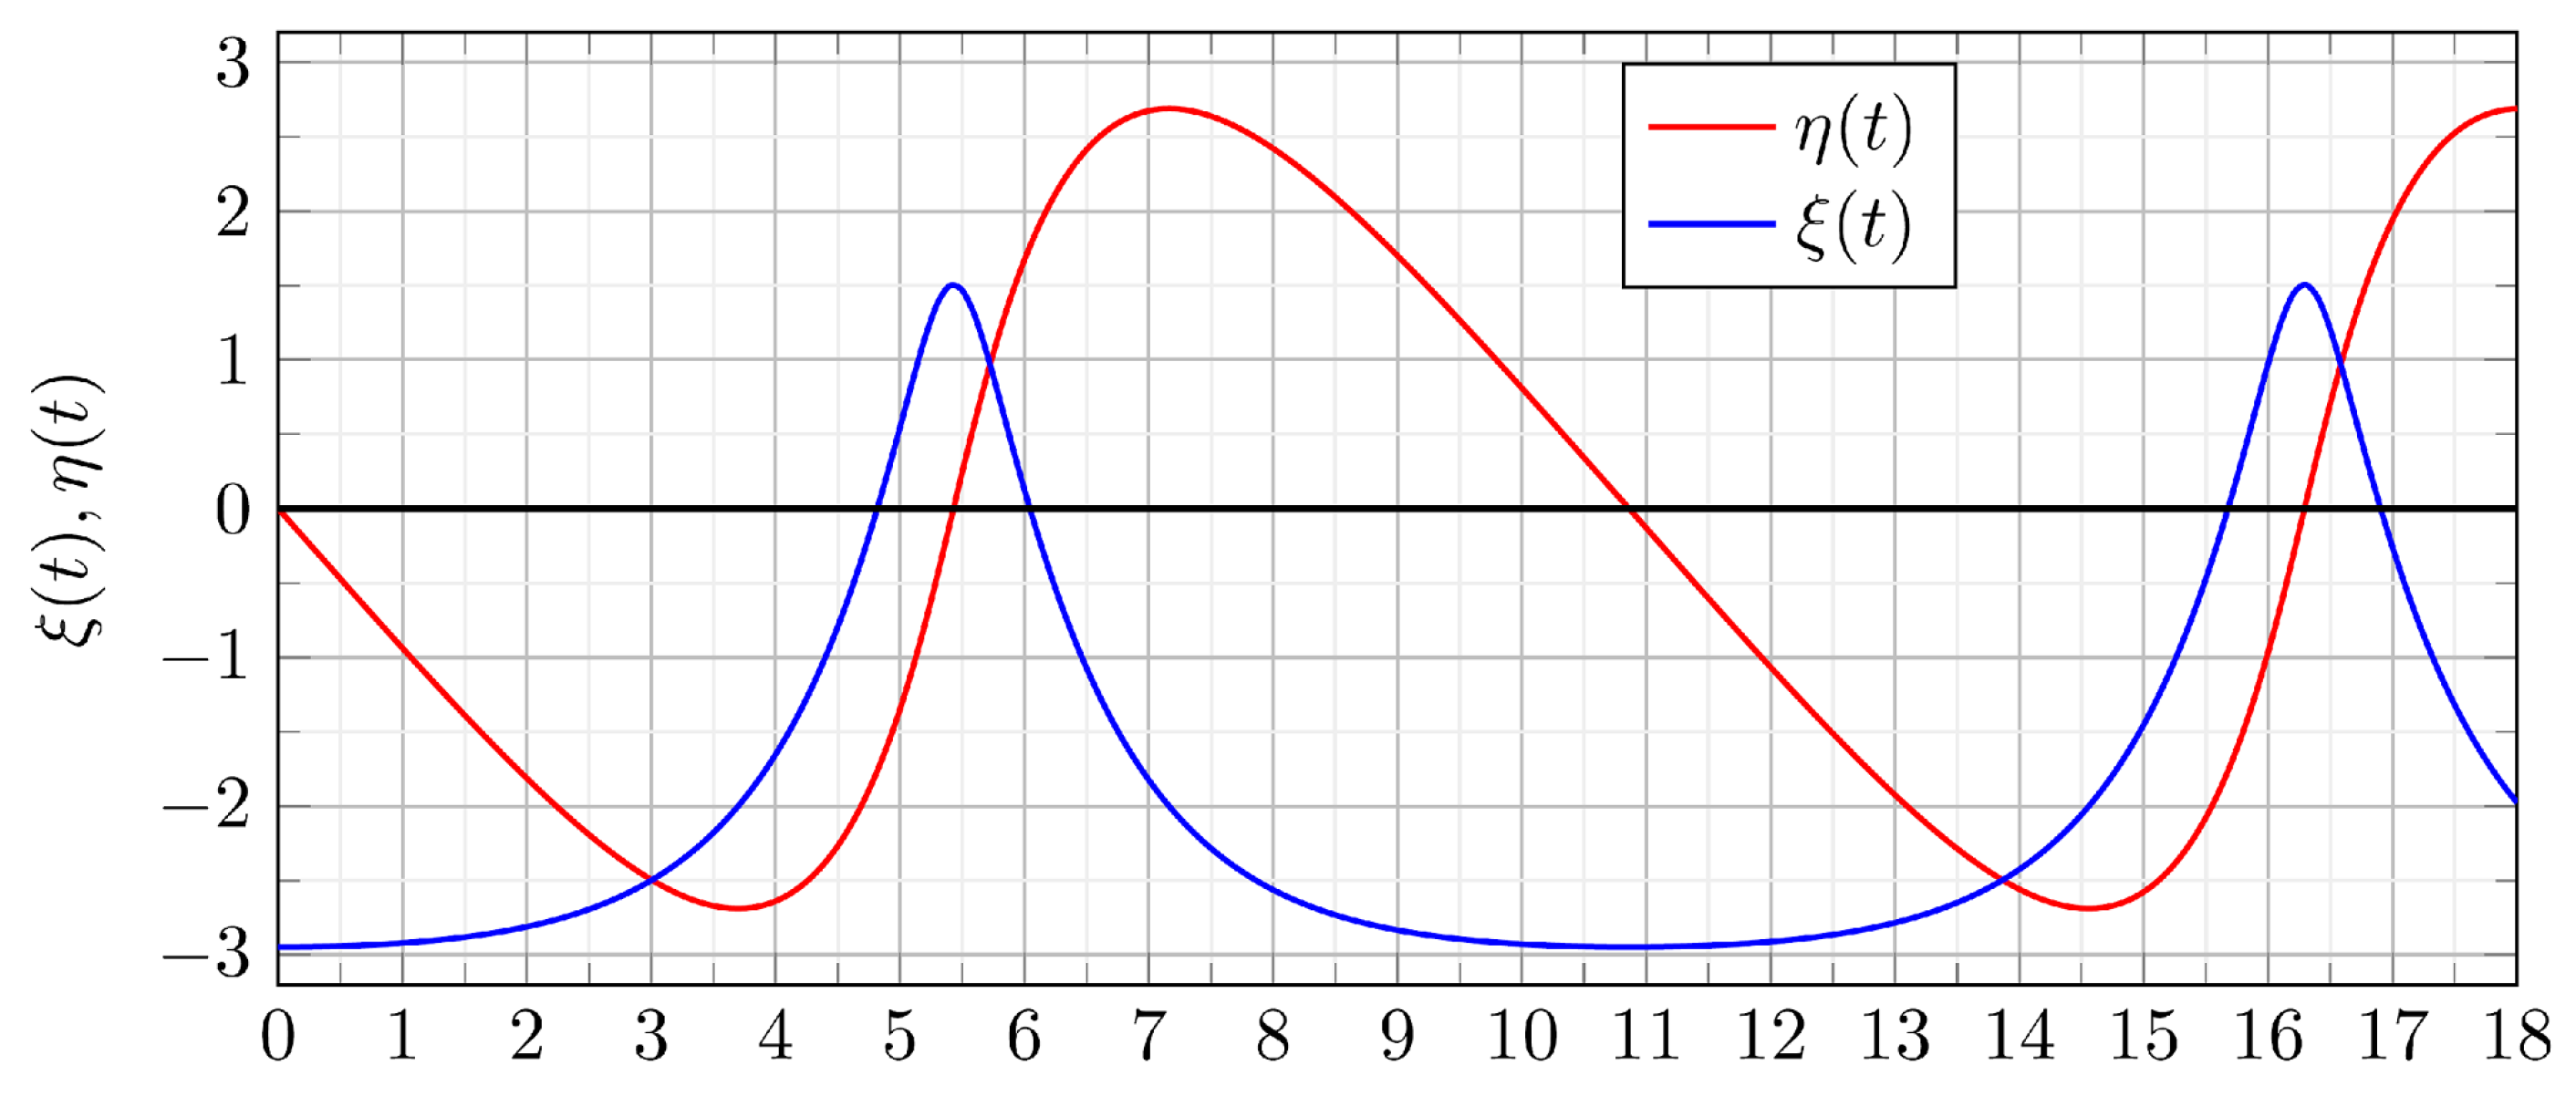
A numerical solution for
can also be obtained by integrating (23b) using a standard fourth-order Runge–Kutta (RK4) method.
Figure 3 presents the
solution obtained by numerical integration for an energy
with initial condition
. The growth and decay phases of the even function
are symmetric relative to the half period
when
(see
Section 5). The LV system solution is finalized for the two branches
by inserting
, derived above, into (
22) since
.
Over the respective intervals
and
corresponding to the growth and decay phases of
, an integral expression for
is readily obtained by performing the integration with the respective positive root (growth phase) and negative root (decay phase) in (23b), yielding the following
quadrature solution:
At the respective turning points and , the integrand of (25) has a square root-type singularity, which is a stiff challenge in numerical integration. Yet, it is strictly continuous over the interval and the improper integral is convergent.
Together with (
22), the exact integral solution (25) for the symmetric function
over the respective growth and decay intervals constitutes the final solution of the LV problem for the hybrid functions in this special
case.
The solution (25) is similar in form to an analytic quadrature solution derived by Evans and Findley (Equation (17) in [
9]); however, the authors do not indicate how to solve their function’s numerical integration since it contains a square root singularity. The integral (25) lends itself to a more natural quadrature solution predicated on (16) and derived in
Appendix A in terms of the bounded Lambert W function, which analytically removes the square root singularity from the denominator. Both integral formulations are equivalent, but the Lambert W substitution provides a justified numerical evaluation scheme.
3.2. Solutions for the Prey and Predator Species Populations in the Case of
Exact solutions for the time evolution of the prey and predator populations are derived by inserting the respective functions
and
obtained from (25) and (
22) into the original definitions (9). This results in two
uncoupled solutions for the original individual prey and predator species populations
and
. Over the growth and decay phases of the
function, these exact
uncoupled analytical solutions are expressed as
Interval ↦ interval
, i.e.,
growth phase
with
derived from (
25a) together with
.
Interval ↦ interval
, i.e.,
decay phase
with
derived from (25b) together with
.
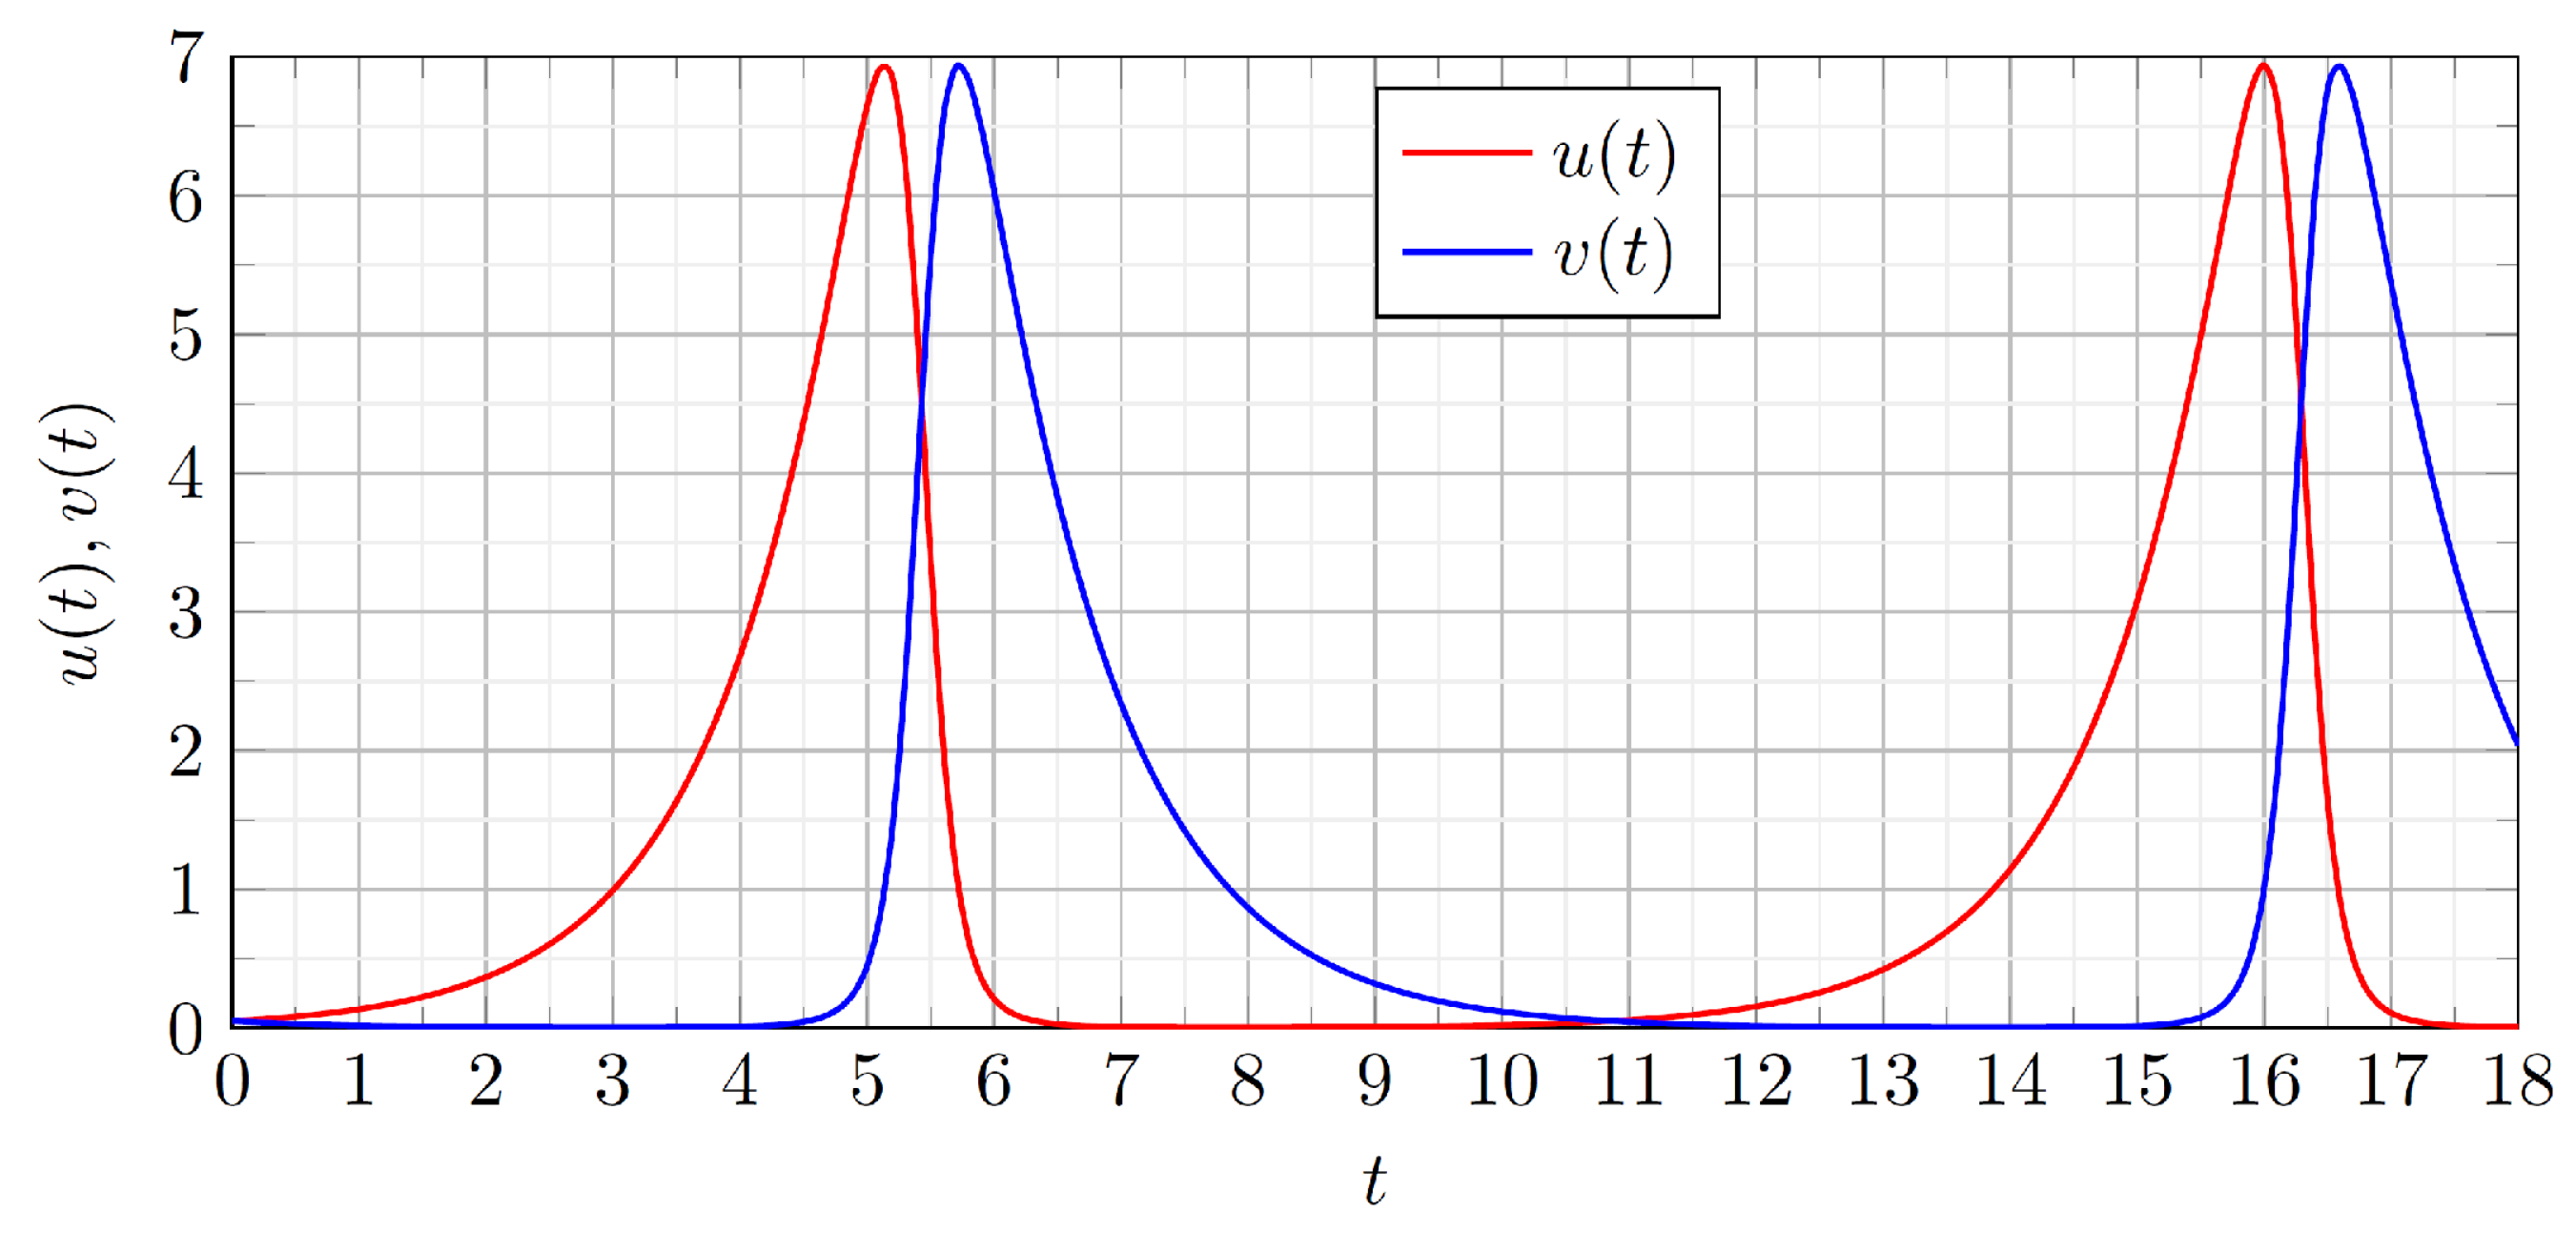
Figure 4 displays the graph of the uncoupled analytic solutions for the time evolution of
and
when their respective growth and decay rates have equal magnitude and when the system’s energy is
. Remarkably, due to the uncoupling in (23), the
and
solutions do not explicitly depend on
.
It is observed that the prey population exhibits an initial growth at a rate significantly slower than its own fast decay rate, while the opposite is the case for the predators; also the peak population of the prey occurs when the population is mature, i.e., when the predator population is relatively small, , and vice versa.
3.3. Case
In the general case when
the relationship between
and its derivative
is obtained by observing that
Upon eliminating
between (
11) and (
28), an implicit nonlinear 1st-order ODE relating
G to its derivative
is derived (for clarity the index
is omitted in the remainder of this section):
Equation (
29) is completely invariant under the change
or equivalently changing
together with
. As a result, similar to (
22), in the
phase space, (
29) represents the positive and negative branches of a “skewed” hyperbola with orthogonal asymptotes, respectively
and
, together with a vertex
G′ = 0 located at
. For any value of
, the function
reaches its extremes at the two roots of
. Also, as expected, in the case of
, (
29) identically reduces to (
22).
Being implicit, (
29) can generally not be solved for
as a function of
G by standard algebraic techniques. A practical yet accurate approximation for the function
predicated on (
20), which removes the
dependence in (17b) and uncouples the system, is proposed below.
For the positive branch
, for large
G, the function
is asymptotic to
. Equation (
29) is first reformulated as
The factor in parentheses in the denominator always satisfies the inequality
Upon approximating this factor by its exponential limit, (
30) becomes
Since the
G function is bounded by
, the right-hand side of (
32) satisfies the following inequalities:
Consistency between (
32) and (
33) requires the left-hand side of (
32) to at most be of order
O(1). Consequently, a Taylor expansion of the exponential function to 1st order can be used, yielding an explicit approximation for
. (The neglected term is the quadratic term
. To estimate the truncation error, the relevant range for
G is the compact interval
, where the last bound corresponds to
, i.e., when
is either minimum or maximum. Near the vertex
,
and
, and the error is second order and small; at the other extremity
, defining the magnitude of the gap between the positive branch of
and its asymptote
as
with
and, if
, then the neglected term is
;
s approaches its extreme value there and diminishes as the gap increases towards the vertex of
G. This is consistent with the visible departure between the approximate and RK4 curves of
Figure 5.) The negative branch
is obtained from the positive branch
G′ ⩾ 0 by
invarianceRemarkably, the above approximate function
satisfies the following three basic properties that are identical to those of an exact numerical solution of (
29):
- 1.
At its vertex, when , the function reaches ;
- 2.
For , as expected, the positive branch of the function is asymptotic to , whereas the negative branch is asymptotic to ;
- 3.
For
, the function
reduces to the exact predicate expression (
20).
In the
phase space, the explicit expressions (34) represent approximate positive and negative branches of the “skewed” hyperbola, defined by (
29), bounded by the same orthogonal asymptotes. Graphic comparison between representations of (34) and a numerical solution of (
29) for
shows quite reasonable agreement consistent with the first two properties of (34), particularly for the positive
branch when
and conversely for the negative branch when
. For
the graph of (34) exhibits two branches bounded by their respective orthogonal asymptotes, with the accuracy of this approximation increasing with increasing
.
As intended, approximation (34) effectively uncouples the system (17) by explicitly removing the dependency on
in the original ODE (17b): upon inserting the conservation Equation (
12) into (34), Equation (17b) is replaced by a pair of two
-
invariant 1st-order autonomous nonlinear ODEs for
corresponding to each
branch of the
closed-form mapping
As
the approximation (34) approaches the exact solution (
20), and, for
, the two branches of (23b) are strictly recovered. Upon choosing the time
when
, a complete oscillation period is obtained by integration over the corresponding negative
branch in (35b) until
reaches
, followed by an integration over the positive
branch (
35a) until
is reached. Even though
is not explicitly expressed as a function of time
t, the arbitrary
problem has thus been reduced to a pair of
simple quadratures for the function
. The approximate function
is monotonic and continuous on the respective integration intervals
and
, and its inverse function
exists and is unique, monotonic, and continuous on each interval.
The LV problem is then completed for the function by directly integrating the linear Equation (17a) through standard numerical techniques.
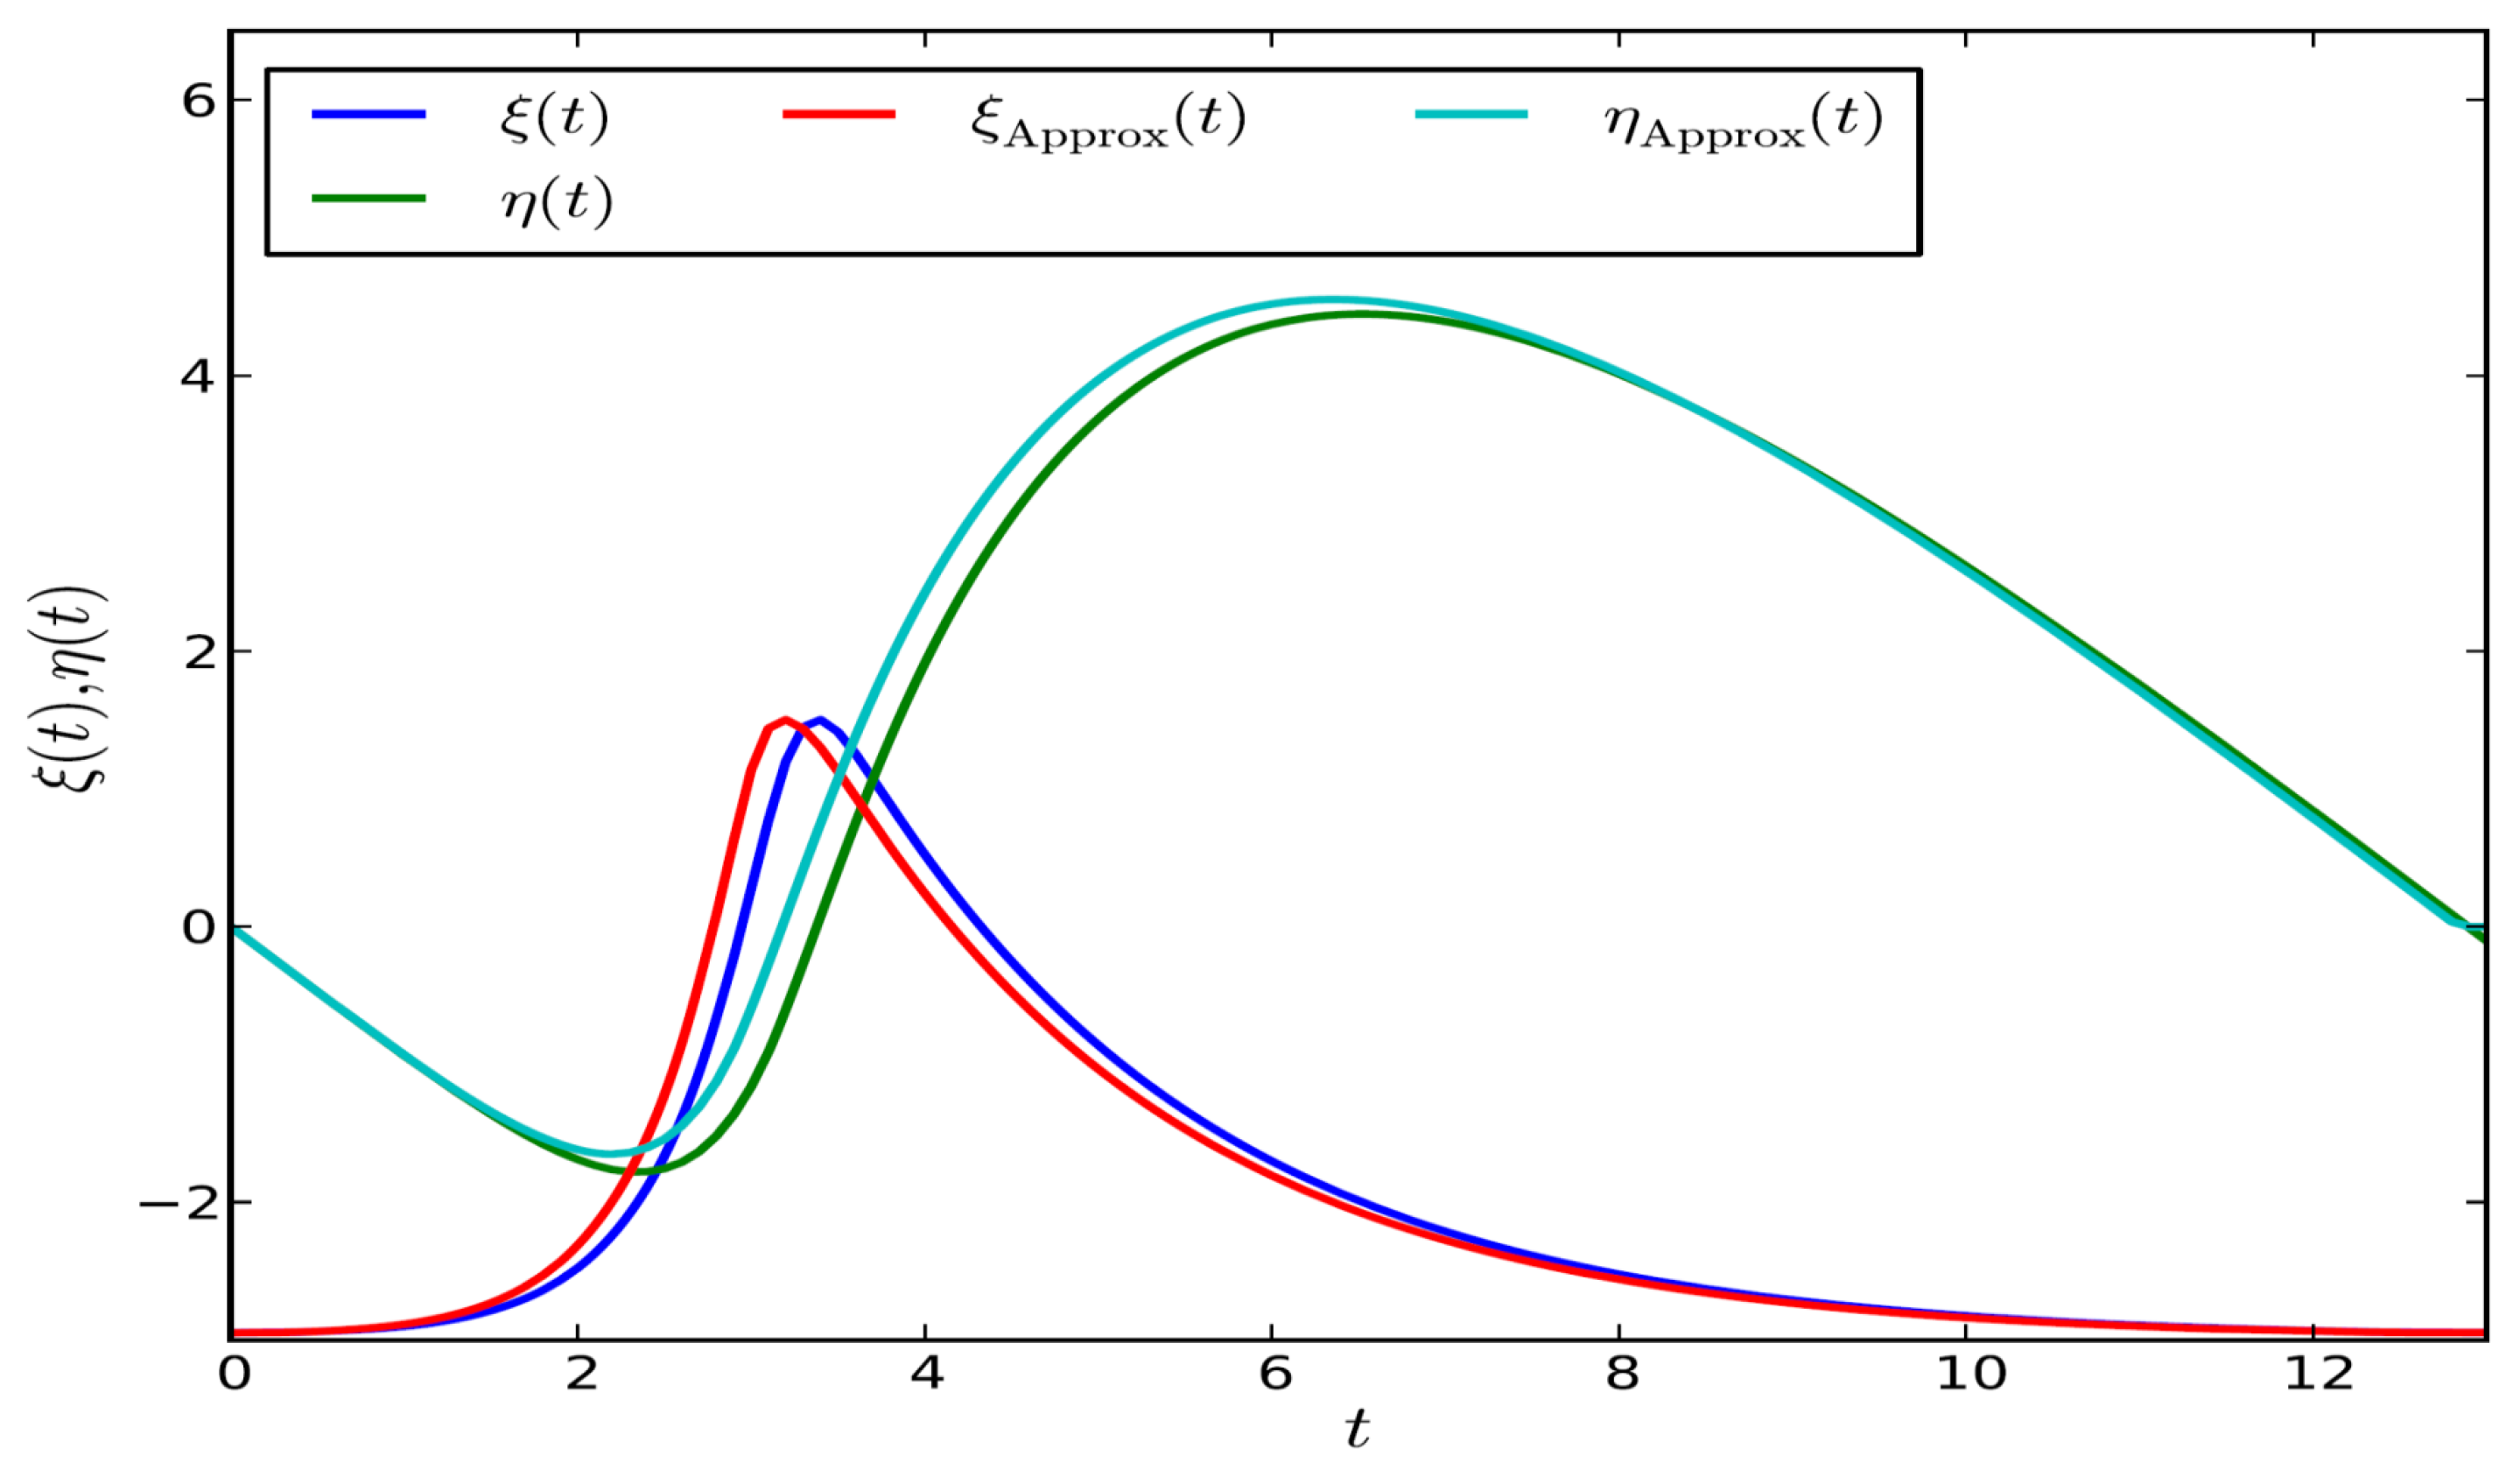
To assess the accuracy of the uncoupled approximate solution (35), a comparison is made with the exact numerical solutions of the original coupled LV system (17). Upon using the respective values
and
, identical to those of
Figure 2,
Figure 5 presents the functions
and
, obtained, respectively, by numerically integrating (35) and (17) simultaneously through a standard 4th-order RK4 method. Despite not being exact solutions, the ODEs (35) provide a reasonably accurate solution for both functions
and
over an entire period. However, when
, an underestimation of the time taken to reach
is compensated by an overestimation of the time to reach
.
As expected, the accuracy of the solutions obtained with approximation (35) increases with increasing
. This can be observed by measuring the mismatch
between the exact
peak amplitude time
and the approximate time
, obtained, respectively, with the RK4 solution and the approximation (35). In
Figure 5, for an energy
and for
, this mismatch is
or 5.80% of
.
Table 1 displays the peak amplitude
together with the period
and the relative mismatch
as a function of
for
. It demonstrates the accuracy improvement of the approximation (35): for a given
h, as
increases, the period increases smoothly, whereas the time
simultaneously diminishes, implying a faster relative growth of
. A similar analysis for
and various values of
h shows that the approximation
stays within 4% of the RK4 solution, but it diverges beyond
since the positive
branch of the approximate function fails to return to 0 in the vicinity of the time
.
Remarkably, in the high-energy limit
, upon keeping the leading term of the approximate system in (35), the asymptotic behavior of the LV system is modeled as a system of two coupled
linear 1st-order ODEs for
and
. In this asymptotic limit, together with the linear ODE (17a) for
, the system admits trivial exponential solutions. For example, the asymptotic solutions
for the growth phase
simply are
The decay phase asymptotic solutions for are obtained by invariance, namely together with .
Lastly, upon inserting the hybrid functions
and
derived from (36) into the definition (5) of the prey and predator species, the respective standard solutions for the original populations
and
are fully recovered,
3.4. Ranges of and h
The oscillation amplitude is mostly associated with the energy h, whereas the respective growth and decay rates and together with the time for peak amplitude of are mostly related to the magnitude of the coupling ratio .
Further, the
and
h ranges for which the approximation (35) is quantitatively acceptable are directly related to the uncoupling of
since, when
, it mostly affects the values of the positive
branch, particularly in the vicinity of
. Hence, as seen above, the energy range is limited to moderate values
. It should be noted that, in the case of
, there is no limit on
h, as shown in
Section 4. Since the coupling ratio mostly affects the growth and decay rates of
in which shorter approximate times
in the growth phase compensate for much longer approximate times during the decay phase, the resulting sum
becomes a smoothly increasing function of
, as shown in
Table 1. Consequently, a moderate limit
is an acceptable range for the coupling ratio. From an ecological viewpoint, this is likely to be a conservative high limit since it implies
, a very high growth rate for prey relative to the predator decay rate.
5. Conclusions
The objective of this research has been to formulate the LV problem into a simple compact form while attempting to uncouple the basic ODE system: the historic LV-coupled first-order nonlinear ODE system of two interacting species has been recast in terms of a single positive coupling parameter , the ratio of the relative growth/decay rates of each species taken independently. A Hamiltonian formulation combined with a linear transformation introducing hybrid variables partially uncouples the system into a -invariant set of two first-order ODEs, with one being linear. This enables to be formulated in terms of a simple integral. As a result, an exact quadrature solution of the LV problem is derived for any value of the coupling ratio and the system’s energy.
In the general case of , an attempt has been made to uncouple the LV system by deriving an approximate ODE for that is autonomous, like in the case of . This has provided accurate practical approximate integral solutions that are not solvable in terms of standard functions. The quantitatively acceptable approximation ranges for the energy h and the coupling ratio are provided. Remarkably, at high orbital energies, the uncoupled system becomes entirely linear, admitting trivial closed-form asymptotic exponential solutions. Further, for any value of the coupling ratio , the oscillation period is shown to be a monotonically increasing function of the energy and of ; at high energies and , a trivial reasonably accurate asymptotic expression for the oscillation period is derived, showing that higher oscillation amplitudes result in longer oscillation periods.
The case, in which the intrinsic exponential growth and decay rates of the predators and prey are equal, represents a genuine, if special, ecological symmetry condition: it is the condition under which invariance becomes a self-duality. As such, through the exact uncoupling (22), together with the simple quadrature (25) expressed in terms of a bounded integral through the Lambert W function and the expansion of the energy function , this case represents a benchmark or limiting case for the accuracy of the approximation.
When
, the LV problem completely uncouples and an
exact explicit solution is derived in terms of the system’s orbital energy as a simple quadrature for the time evolution of one of the hybrid functions, the solution for the other function being explicitly expressed in terms of the former. Predicated on the exact closed-form energy-dependent turning-point solutions, this basic quadrature is restructured in terms of the Lambert W function, which eliminates the square root singularity but shifts the burden to the delicate exercise of accounting for the ill condition of the Lambert function near its branch point.
Appendix A establishes that the integral is regular at the branch point but must be evaluated numerically. Also, exact
uncoupled analytic solutions for each of the original prey and predator populations are derived as a function of
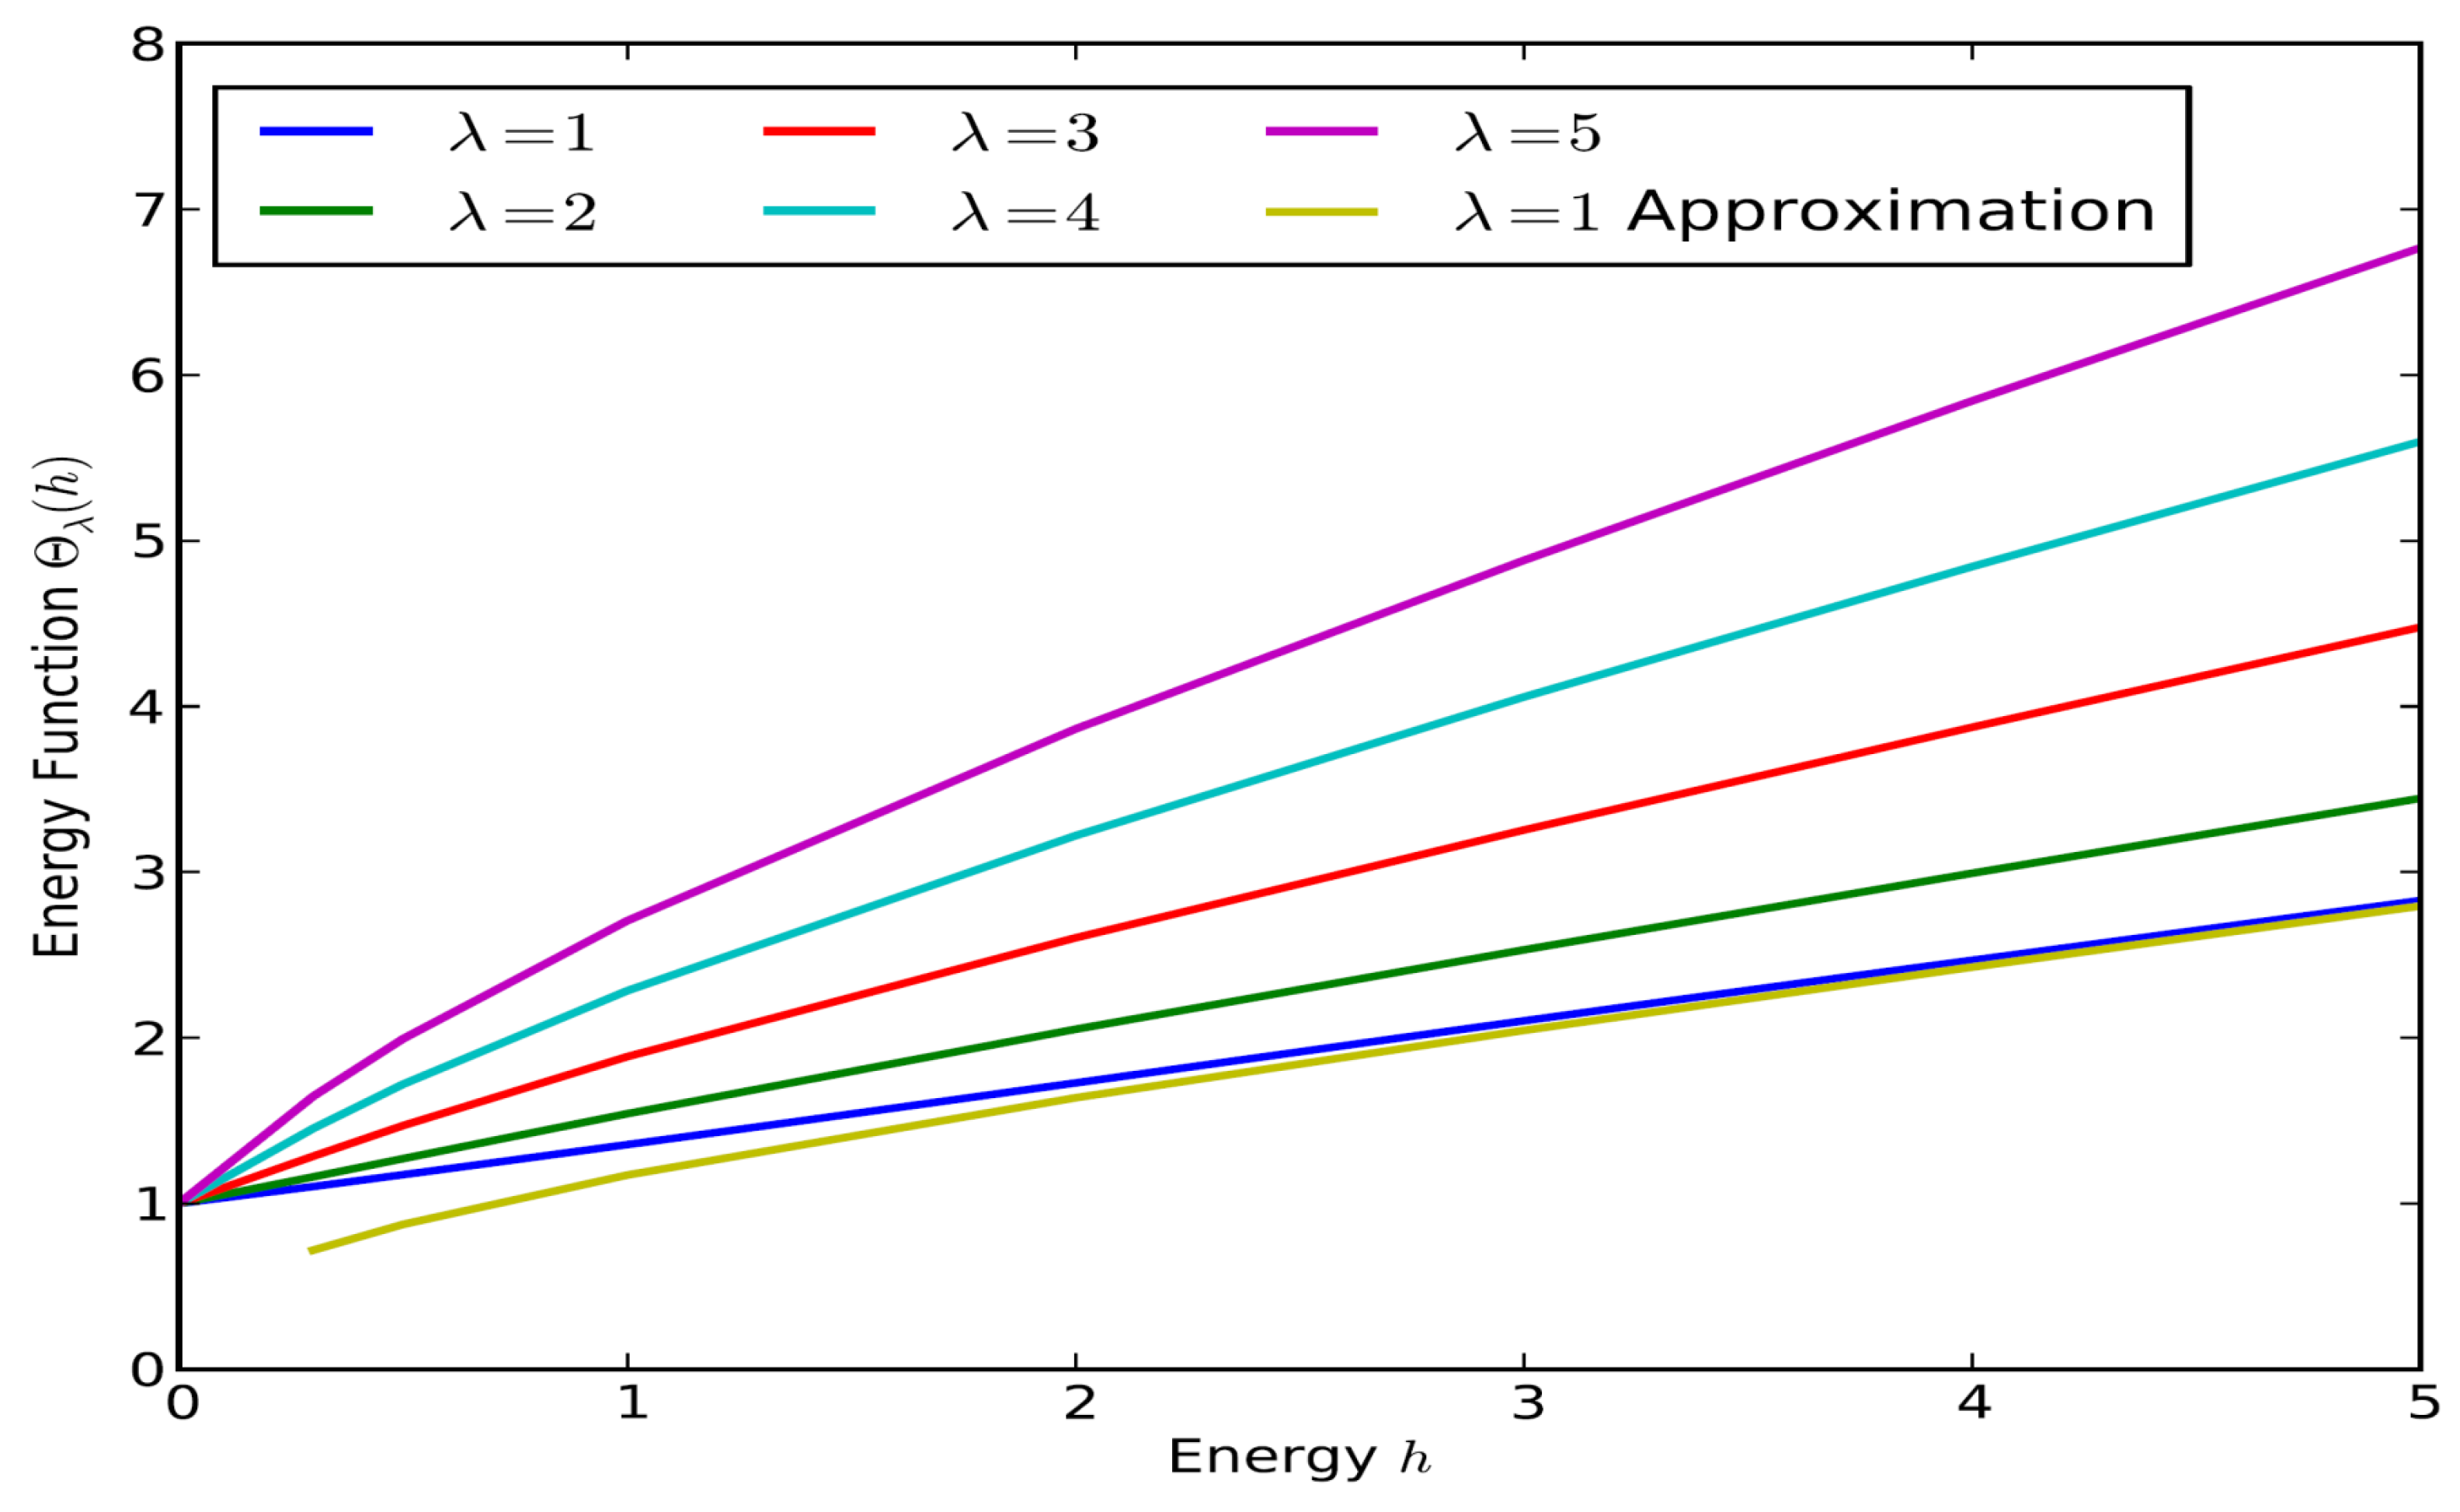
. Lastly, an exact analytic expression for the LV system oscillation period is derived in terms of a dimensionless energy function together with a simple closed-form asymptotic expression for high energies.
This research highlights several areas that warrant further investigation: (1) not unlike several other authors, due to the particular nonlinearity in the coupling of the LV problem, compact solutions for the evolution of the predators and prey are expressed in terms of quadratures only except in the case of asymptotic solutions; (2) the uncoupling is only an approximation, yet it is reasonably accurate for moderate energy values; (3) even though predicated on the closed-form solutions for turning points, the Lambert W function representation does not yield a full solution in terms of standard functions, although it eliminates the square root singularity in an integral that poses a stiff numerical integration challenge.
Nevertheless the paper presents valuable contributions: (1) the Hamiltonian formulation for hybrid variables and and the invariance, as well as reducing the system to two ODEs, with one being linear (which is not the case in the LV system) and, in the case of , the second being autonomous, thereby providing structural insight into the LV problem; (2) exact closed-form solutions for the turning points are expressed in terms of the Lambert W function; (3) the numerical figures (RK4 vs. quadrature approximate solutions) are consistent with the stated accuracy; (4) the case, which may be perceived as too narrow, particularly from an ecology standpoint even though it provides exact closed-form mapping and quadrature solutions, is shown to fold in the general approximate uncoupling case; (5) formulae for the period are expressed as simple integrals over the mapping and not as convolution integrals that are more difficult to evaluate numerically; (6) useful asymptotic closed-form expressions for , and are also derived.