Review

Bioactive Properties and Pharmaceutical Potential of New World Mistletoes of the Genus Tristerix: A Review


by
Erick Poulsen-Silva
1,
María Carolina Otero
1,
Diego Verdugo-Igor
2,3,
Gloria González
2,
Sofía Díaz-Cornejo
4,
Camila Fuentes
5,
Maite Rodríguez-Díaz
6,
Cristian Atala
7 and
Felipe Gordillo-Fuenzalida
4,*
1
Escuela de Química y Farmacia, Facultad de Medicina, Universidad Andres Bello, Santiago 8370035, Chile
2
Laboratorio de Patomolecular y Biocompuestos, Centro de Biotecnología de los Recursos Naturales (CENBio), Facultad de Ciencias Agrarias y Forestales, Universidad Católica del Maule, Avda. San Miguel 3605, Talca 3480112, Chile
3
Doctorado en Biotecnología Traslacional (DBT), Universidad Católica del Maule, Avda. San Miguel 3605, Talca 3480112, Chile
4
Laboratorio de Microbiología Aplicada, Centro de Biotecnología de los Recursos Naturales (CENBio), Facultad de Ciencias Agrarias y Forestales, Universidad Católica del Maule, Avda. San Miguel 3605, Talca 3480112, Chile
5
Programa de Doctorado en Ciencias Agrarias, Facultad de Ciencias Agrarias, Universidad de Talca, Talca 3460000, Chile
6
Carrera de Química y Farmacia, Facultad de Ciencias Naturales, Matemáticas y Medio Ambiente, Universidad Tecnológica Metropolitana, Santiago 7780125, Chile
7
Laboratorio de Anatomía y Ecología Funcional de Plantas (AEF), Facultad de Ciencias, Instituto de Biología, Campus Curauma, Pontificia Universidad Católica de Valparaíso, Av. Universidad 330, Curauma, Valparaíso 2340000, Chile
*
Author to whom correspondence should be addressed.
Sci. Pharm. 2026, 94(3), 66; https://doi.org/10.3390/scipharm94030066
Submission received: 31 May 2026 / Revised: 25 July 2026 / Accepted: 5 August 2026 / Published: 7 August 2026
(This article belongs to the Topic Natural Products and Drug Discovery—2nd Edition)

Abstract

Mistletoes of the genus Tristerix, native to South America, represent a unique group of mostly hemiparasitic plants with potential medicinal applications. This review synthesizes existing knowledge on their biological and phytochemical properties, focusing on three main species endemic to Chile: Tristerix aphyllus, T. corymbosus, and T. verticillatus. These species exhibit diverse interactions with host plants, animal pollinators, and seed dispersers, where host identity can influence their chemical profile. Around 17 metabolites have been found in flowers, fruits, and leaves from Tristerix spp., including flavonoids (e.g., quercetin, apigenin, luteolin), phenolic acids (e.g., caffeic acid; gallic acid), and alkaloids (e.g., pronuciferine and glaucine). Those have demonstrated antioxidant, anti-inflammatory, antimicrobial, and anti-tumoral properties. Despite their traditional uses in Chilean medicine for ailments such as gastric ulcers and throat infections, experimental research on Tristerix spp. remains scarce. This review highlights their bioactive potential, emphasizing the need for further investigation into their pharmacological applications, including in vivo and clinical studies.

Graphical Abstract

1. Introduction

The use of medicinal plants in ancestral cultures has been the basis of present-day pharmaceutical prescriptions, and the country of Chile is no stranger to the use of native botanical species in various applications [1,2]. Chilean endemic plants have garnered significant research attention due to their unique properties and conservation importance. With a diverse climate that incorporates temperate rain forests, deserts, and mountainous and marine regions, the Chilean territory is the source of over 80 genera of endemic plants, with the southern regions harboring more phylogenetic diversity than expected [3,4]. Several indigenous groups from Chile, such as the Mapuches people, have used this traditional knowledge for centuries, which include the use of various plant species for medicine, food, crafting, cosmetics, and rituals, among other uses. To this day, this kind of documented data are still being researched to fully understand the biological properties of these natural sources and the impact that they caused in their culture [5].
A particular group of plant species that have received attention belongs to the family Loranthaceae, commonly known as New World mistletoes, which comprises approximately 1000 species distributed across 77 genera [6]. This family is composed of mostly hemiparasitic plant species [7], presenting photosynthetically active organs (usually green leaves), while receiving nutrients and water from the host with their specialized roots called haustoria, which are connected to the xylem of the host plant [8,9].
In Chile, this family is represented by the genera Notanthera, Desmaria, Ligaria, and Tristerix; with the latter being the most diverse, including three species: T. aphyllus, T. corymbosus, and T. verticillatus [10]. Species of Tristerix occur primarily in the Andean regions of South America, reflecting their adaptation to high-altitude environments [7]. Members of this genus are characterized by their distinctive red flowers [9]. They are pollinated mainly by hummingbirds, whereas seed dispersal is mediated by native and endemic birds and marsupials [11,12]. As noted above, Tristerix species have long been used in traditional medicine by indigenous and local communities for the treatment of various ailments [5,9,13].
Leaves, flowers, and fruits of T. corymbosus are used as pigments, astringents, for treating gastric ulcers and sore throats, and lowering blood cholesterol [12]. Fruits of Tristerix are edible, with a sweet taste, but are consumed mostly in rural areas [9,13,14,15]. Fruits and other organs of T. corymbosus and T. verticillatus can be used as a natural black pigment for staining [9,16]. However, studies regarding its biological properties are few, and most of them are focused on determining their phytochemicals to give support to their medicinal properties [17,18]. Furthermore, there are no studies performed on in vivo models, not even clinical studies in order to demonstrate safety of these extracts.
This lack of proper research is relevant since the genus Tristerix, and its family Loranthaceae, are part of the Santalales order, which incorporates a broad number of different species, including the genus Viscus, commonly known as mistletoes. These species of hemiparasitic plants have been used in traditional medicine around the globe for centuries, with well-documented studies on their anti-inflammatory, antibiotic, antioxidative, antihypertensive, hepatoprotective, neuroprotective, anti-tumoral, and immunomodulatory properties; even to the point that standardized preparations of compounds found on Viscus album L., mainly lectins and viscotoxins, are available commercially for the treatment of cancer [18,19].
In this narrative review, we examine the botanical characteristics and analyze the bioactive properties of the genus Tristerix, along with its chemical composition. A narrative approach was considered appropriate due to the limited and highly heterogeneous literature available regarding Tristerix spp., particularly concerning their ethnobotanical uses, phytochemistry, and biological activities, which precludes a systematic quantitative synthesis. Here, we compile the reliable information available to assess its potential for pharmaceutical use, including ethnobotanical records and experimental studies that highlight its medicinal applications.

2. Material and Methods

This study was conducted as a narrative review to synthesize the fragmented and heterogeneous data surrounding the genus Tristerix. To ensure methodological transparency and reproducibility, the literature search and study selection were guided by the following parameters:
Rationale for Database Selection: The scientific literature search was performed using NCBI-PubMed, Google Scholar, and Mendeley databases. These platforms were selected due to their comprehensive coverage of biomedical, chemical, and multidisciplinary Latin American scientific literature, which is essential for capturing studies on regional endemic flora.
Search Strategy and Time Frame: The search covered articles published over a 38-year period from 1986 to 2024. Search strings utilized combinations of Boolean operators and the following keywords: (“T. aphyllus” OR “T. corymbosus” OR “T. verticillatus”) AND (“antioxidant property” OR “antioxidant activity” OR “antimicrobial property” OR “antimicrobial activity” OR “anti-inflammatory property” OR “anti-inflammatory activity”).
Language Restrictions: The search was limited to articles published in English and Spanish, considering that a significant portion of ethnobotanical and historical data on Chilean native plants are documented in local Spanish-language journals.
  • Inclusion and Exclusion Criteria:
Inclusion criteria: Peer-reviewed original research articles, short communications, academic theses, and botanical field guides that provided direct experimental data (in vitro, in vivo, or phytochemical profiling) or documented ethnobotanical uses of the specified Tristerix species.
Exclusion criteria: Studies focused exclusively on other Loranthaceae genera without comparative data for Tristerix, non-peer-reviewed blog posts, conference abstracts lacking full data, and duplicates.
In order to enhance this narrative review, a patent search was performed through Google Patents, Espacenet, and WIPO PATENTSCOPE. Scientific names Tristerix, T. aphyllus, T. corymbosus, and T. verticillatus, as well as relevant taxonomical synonyms, were used as keywords in the search process. In addition, other keywords relating to bioactive compounds and their applications, like extract, phytochemical, pharmaceutical, nutraceutical, and antioxidant, were searched.
Chemical structures were redrawn using MarvinSketch (ChemAxon, version 17.14) based on structural information available in the PubChem and ChemSpider databases.

3. Results and Discussion

3.1. Botanical Characteristics, Ecology, and Host Association of Tristerix Species

Tristerix species, commonly known as South American mistletoes, are found in South America, particularly in countries like Argentina, Chile, Colombia, Ecuador, and Peru. The Chilean species are characterized by racemose inflorescences bearing bright red flowers, which may also exhibit a golden-yellow coloration in some species. Flowers are tubular, commonly associated with bracts, and with yellow stamens. Leaves are green, usually glabrous, and ovate to narrowly lanceolate in T. corymbosus and T. verticillatus, but absent in T. aphyllus [9]. Pollination is aided mainly by birds, primarily hummingbirds, while its edible fruits are eaten by birds and mammal species [7,18]. Fruits are ovoid berries, usually yellow (in T. corymbosus and T. verticillatus) to light pink (in T. aphyllus). Fruit dispersers can be found perched atop trees or shrubs; these animals then release seeds in their droppings. Seeds are covered in a sticky substance that allows them to hold on to branches and/or leaves of the host plant. Then, it germinates and a petiolar tube emerges, ending in a haustorial holdfast that attaches to branches and initiates parasitism. If the seed cannot find any living branches within a certain time (or a compatible host in some cases), the parasite dies. In most species, the haustoria penetrates the cambial layer and connects itself to the xylem of the host [8].
Tristerix species, unlike some other genera such as Desmaria, usually infect a wide range of host species [20], and the host identity can influence the biochemistry of the parasite; for example, modifying the composition of emitted volatiles [21]. Some of these species have developed a parasitic association to certain host plants, most of them of native origin, which include Aristotelia chilensis (Elaeocarpaceae), Peumus boldus (Monimiaceae), Rhaphithamnus spinosus (Verbenaceae), Luma apiculata (Myrtaceae), and even cacti plants such as Echinopsis chiloensis (Cactaceae). Tristerix spp., particularly T. corymbosus, can also parasite a wide range of introduced woody species such as Populus nigra (Salicaceae) and Acacia spp. (Fabaceae) [7,9].
T. aphyllus is one of the few species that is holoparasitic, lacking photosynthetic tissues and relying on its host for sugars and water [9]. Its main hosts are native cacti, the most common being Leucostele chiloensis (Cactaceae) (Table 1). It is pollinated, as mentioned above, by the hummingbird Sephanoides sephanoides, and its seeds are mainly dispersed by Mimus thenca, another native bird [22,23,24]. Being holoparasitic, the reproductive structures (inflorescence and fruits) are the only portion of the plant that is visible outside their host. This parasitic interaction negatively impacts the health of their hosts, directly affecting their fitness [25,26].
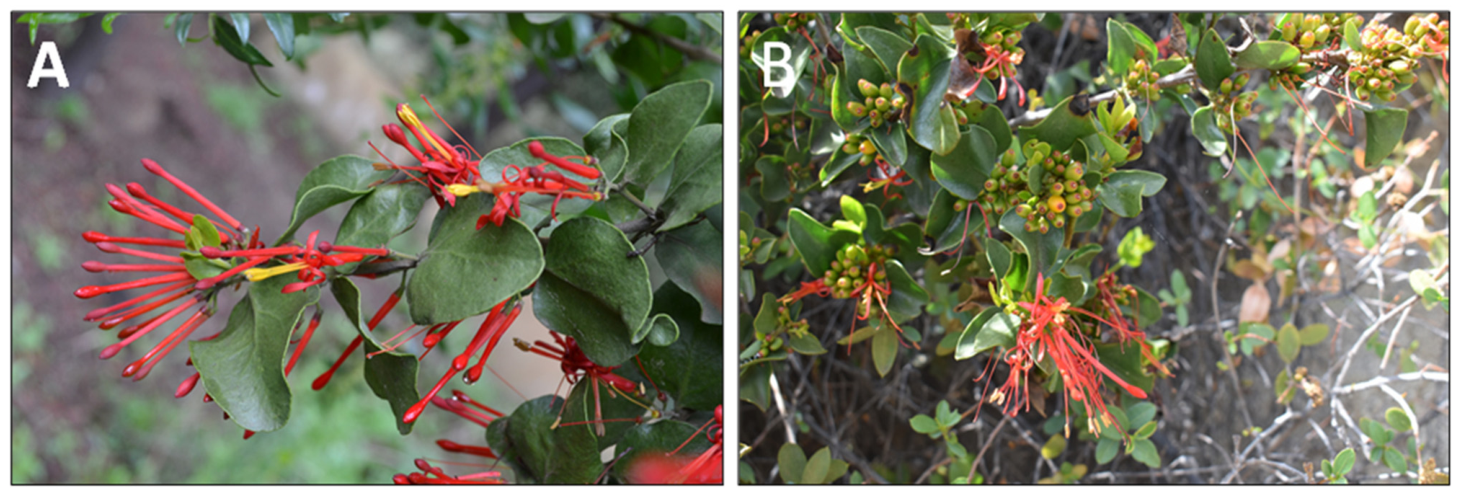
As mentioned before, T. corymbosus and T. verticillatus are both hemiparasitic, featuring green leaves capable of performing photosynthesis (Figure 1). Both species are pollinated by the same hummingbird species as T. aphyllus. Their fruits are dispersed not only by Mimus thenca and other bird species but also by Dromiciops gliroides, an endemic marsupial of Chile and Argentina [31,32,33]. These species are capable of infesting different hosts, mainly native shrubs and trees (Table 1). T. corymbosus, additionally, parasites non-native trees such as Populus and Acacia species, as previously mentioned [7,9,11]. Moreover, it has been suggested that this keystone species could negatively impact invasive tree species and indirectly benefit native species, providing a resistance to invasion in natural ecosystems in Chile [34].

3.2. Phylogenetic Relationships of Chilean Tristerix Species

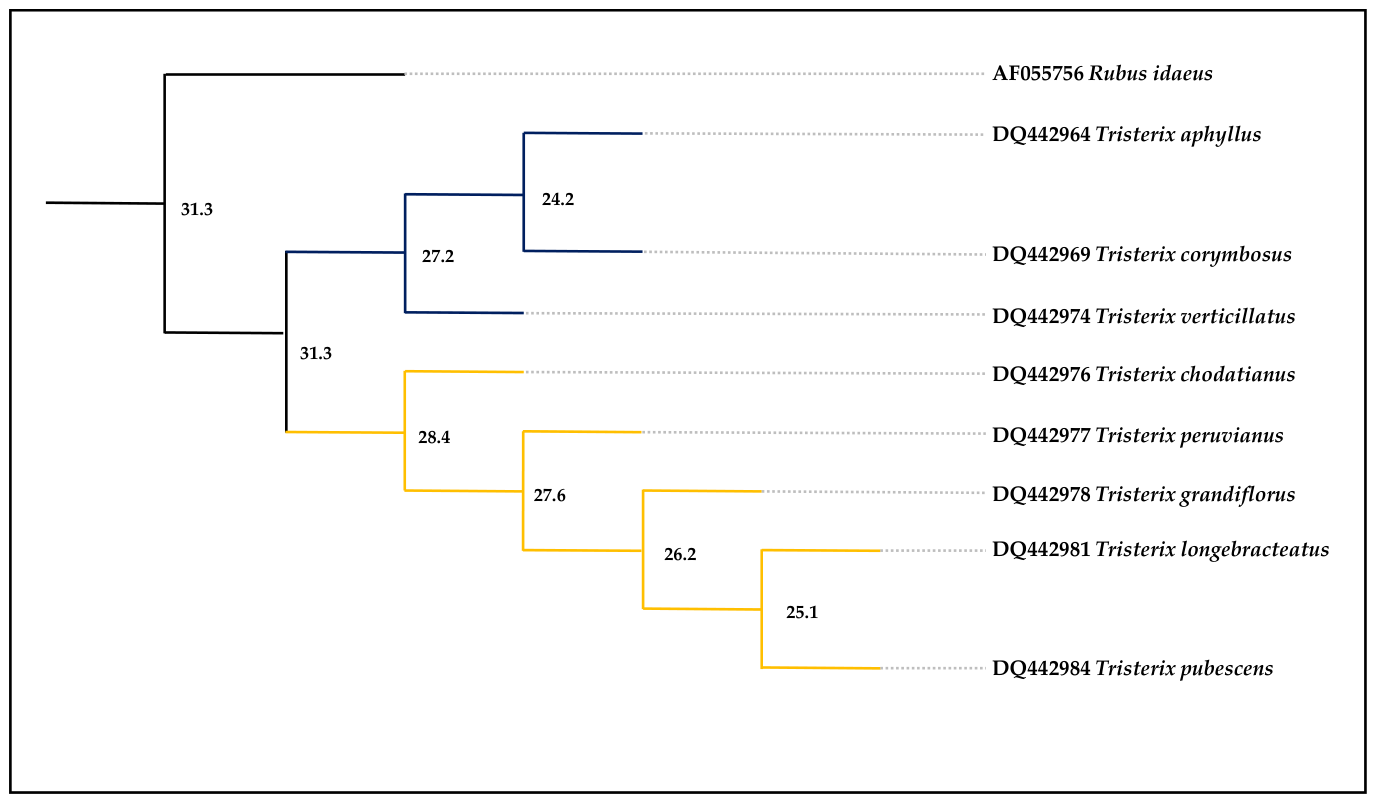
Beside the taxonomic treatment of the Loranthaceae, Chilean species seem to be well-defined and form clear, separate systematic groups. This may have an impact on their phytochemical profiles, not considering the effect of their hosts [35]. When an ITS-based dendrogram is performed using sequences present in databases, two clusters are visualized (namely A and B) which present a 31.3% distance with the outgroup. Cluster A (in blue color) is integrated by a subgroup composed of accession numbers DQ442964 and DQ442969 (with a distance of 24.2%), with a difference of 27.2% regarding accession DQ442974 (Figure 2). On the other hand, Cluster B (yellow) comprises a subgroup of accessions with a mean genetic distance of 26.8%. These results suggest that the division in two clusters could suggest the presence of a separation due to species evolution according to geographic location. Cluster A corresponds to species with a more meridional (Mediterranean–oceanic climates) geographic location, while cluster B groups species with a location around the tropic of Capricorn (tropical climates). Chilean species (T. aphyllus, T. corymbosus, and T. verticillatus) form a separate clade from other South American species. Within this clade, T. aphyllus and T. corymbosus are more closely related, and this may indicate that these species share evolutionary similarities that could be reflected in aspects of their secondary metabolism, although this hypothesis requires phytochemical confirmation.

3.3. Chemical Constituents of Tristerix spp. Extracts

One study used samples of T. tetrandus leaves and flowers to identify metabolites using UHPLC-PDA-HESI-Orbitrap mass spectrometry. They identified a total of 36 metabolites (28 found in leaves and 6 in flowers), with some having well documented antioxidant properties such as chlorogenic acid, catechin, rutin, quercetin-3-O-glucose, quercetin-3-O-pentose, 5-O-caffeoylquinic acid, cyanidin-3-glucoside, malvidin, quercetin, luteolin, naringenin, and apigenin, among others tentatively identified. From these, only malvidin was identified in flowers [36]. Torres et al., determined the qualitative presence of several metabolites from leaves and flowers in different extracts (hexane, dichloromethane, ethyl acetate, and methanol) of T. corymbosus parasitizing Populus nigra (Salicaceae), Aristotelia chilensis (Elaeocarpaceae), and Rhaphitamnus spinosus (Verbenaceae). Tannins, flavonoids, steroids, quinones, saponins, triterpenes, and cardiac glycosides were found. Leaves and flowers of T. corymbosus presented different contents of these metabolites, which could be due to its presence in different hosts [37].
Cifuentes-Araya et al., investigated the application of nanofiltration as a green separation strategy for the recovery of bioactive compounds from T. tetrandus fruits. Using three nanofiltration membranes with different molecular weight cut-offs, followed by UHPLC-ESI-MS/MS analysis, the authors successfully separated and identified several phenolic compounds, including chlorogenic acid, cryptochlorogenic acid, caffeic acid, p-coumaric acid, gallic acid, rutin, and quercetin [38]. Other studies have demonstrated the composition of phenolic compounds across three fractions isolated from the flowers (esterified, free, and insoluble fractions). The esterified fraction contained a significant number of phenolic compounds, including chlorogenic acid, coumaric acid, and sinapic acid [39].
The work of Alarcón-Acuña, studied the phytochemical composition of ethanolic extracts of T. chodatianus leaves (a species infecting Polylepis spp. in Peru). Through various biochemical reaction tests on different fractions of the ethanolic extracts, phytochemical compounds such as phenolic acids, flavonoids, triterpenes, steroids, leucoanthocyanidins, and saponins were found [40].
In 2009, the translocation of alkaloids to T. verticillatus from its hosts was evaluated by comparing the alkaloid content of T. verticillatus hosted by an alkaloid-containing species, Berberis montana (Berberidaceae), a genus known for the presence of isoquinoline alkaloids, and an alkaloid-lacking Schinus montanus (Anacardiaceae) species. The alkaloids pronuciferine and glaucine, which were also found in the host B. montana, were found in T. verticillatus leaves [41].
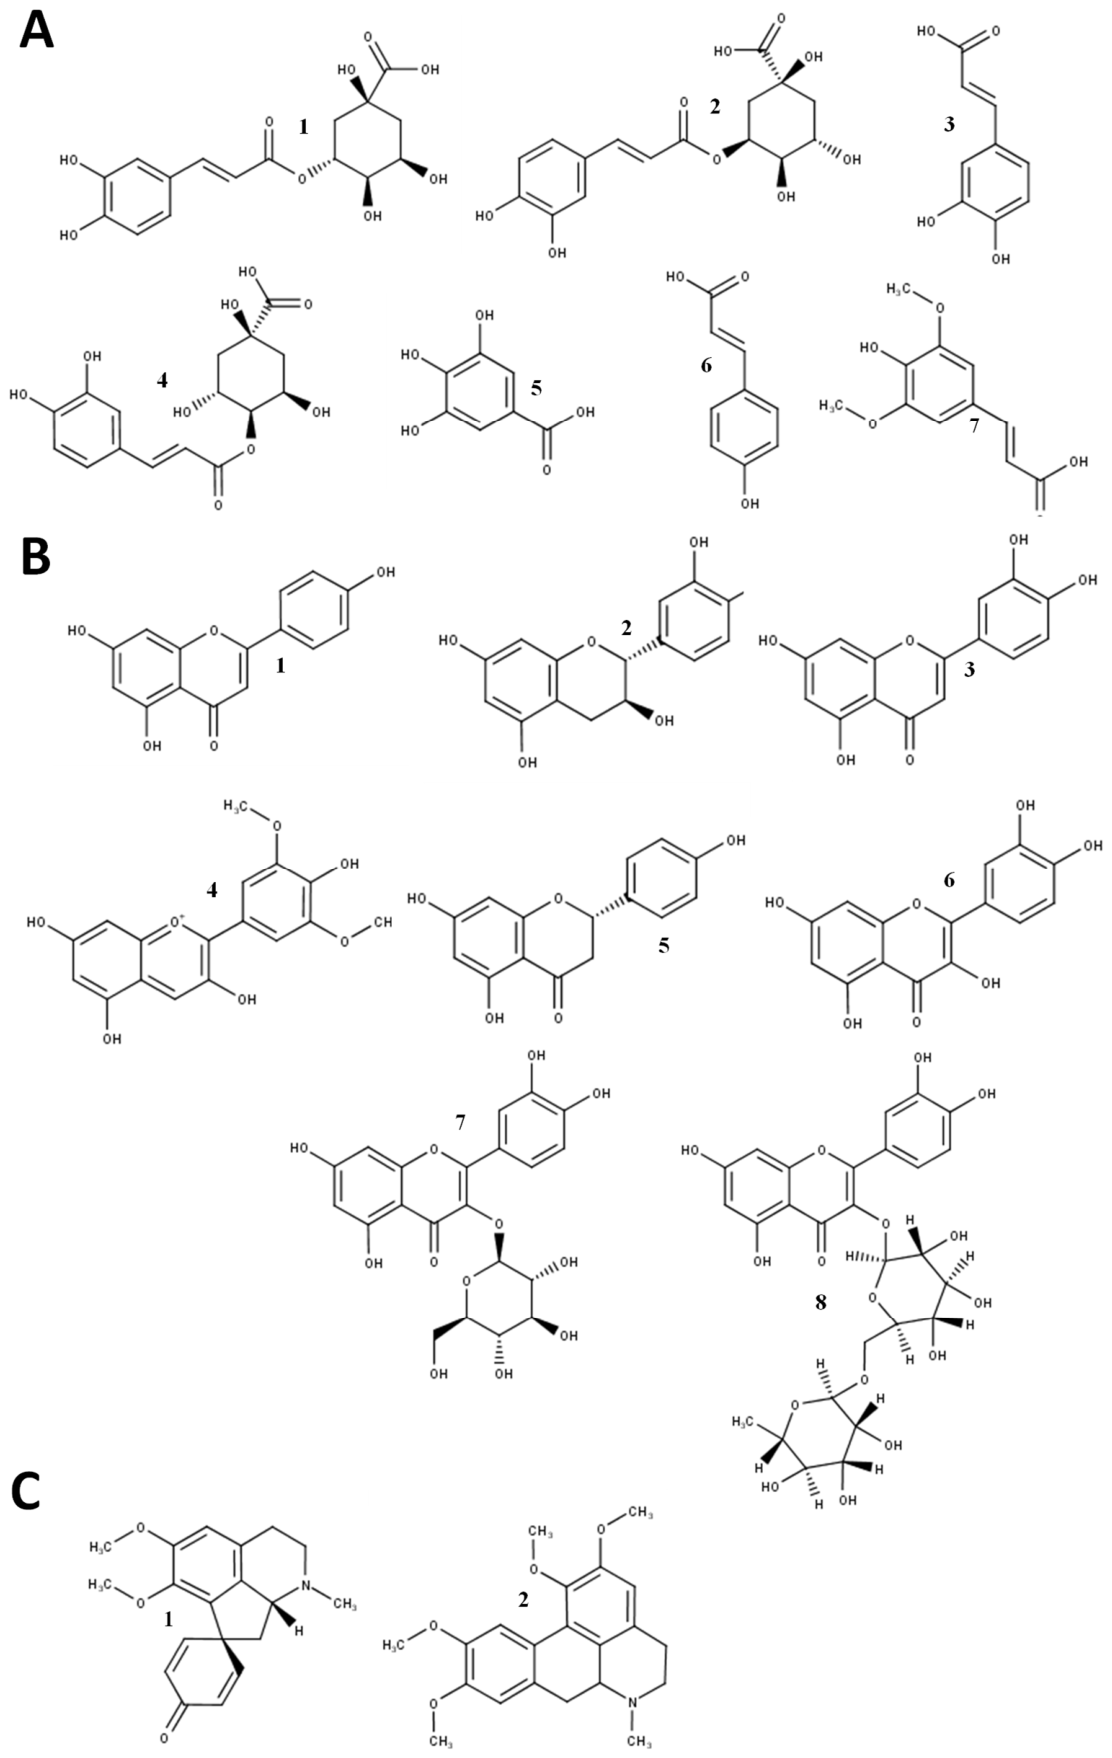
To facilitate comparison among the available phytochemical studies on Tristerix species, the main characteristics of each investigation are summarized in Table 2. The table compiles information on the species studied, plant material, extraction procedures, analytical techniques, major identified metabolites, collection site (when reported), and corresponding references, providing an integrated overview of the current phytochemical knowledge on this genus. Figure 3 summarizes the metabolites reported in the aforementioned studies.

3.4. Biological Properties of Tristerix spp. Extracts

3.4.1. Antioxidant Properties

The study of Simirgiotis et al., evaluated the antioxidant properties of flower and leaf extracts of T. tetrandus with 2,2-diphenyl-1-picrylhydrazyl radical scavenging assay (DPPH), showing that the leaves possess a higher antioxidant activity in comparison with the flowers, which coincides with their higher phenolic and flavonoid content. Ferric reducing antioxidant power (FRAP) assays were also performed on each extract, with flower extracts showing a higher reducing power in comparison. This result also correlates with the flowers’ total anthocyanin content. It is also worth mentioning that the results of the leaves in this assay were comparable with the results obtained from an anthocyanin standard sample of cyanidin-3-glucoside [36].
The study of Torres et al., determined the reductive powers of extracts of T. corymbosus samples from the three different hosts. The extracts were made using different solvents of different polarities, and the solvent that produced the highest yield of extract was methanol. Tristerix leaf extracts from R. spinosus host showed higher reducing power, predominantly the methanol extracts; as well as ethyl acetate extracts of Tristerix flowers parasitizing A. chilensis and R. spinosus. Interestingly, each host resulted in extracts with different contents of secondary metabolites, varying with the presence of flavonoids, phenols, quinones, triterpenes, and glycosides, among others [37]. Besides, in the study of Velásquez et al., the different fractions obtained (esterified, free, and insoluble fractions) exhibited antioxidant capacity against FRAP, DPPH, and 2,2′-azino-bis(3-ethylbenzothiazoline-6-sulfonic acid) (ABTS) radical cation decolorization assay [39].
In the work performed by Alarcón-Acuña, the antioxidant activity of ethanolic extracts of T. chodatianus leaves was assayed. Antioxidant assays such as DPPH and FRAP resulted in a dose-dependent activity in both tests, with a IC50 value of 0.242 mg/mL for the DPPH assay and a Trolox equivalent antioxidant capacity (TEAC) value of 0.642 + 0.008 mg/mL for the FRAP assay [40].

3.4.2. Antimicrobial Properties

In the work of Velásquez et al., the free and esterified fractions presented antibacterial capacity against Escherichia coli, Salmonella enterica serovar Typhy, and Staphylococcus aureus. Chlorogenic and sinapic acids were correlated with the antibacterial capacity against E. coli and S. typhi, while coumaric acid were correlated with the antibacterial capacity against S. aureus. These findings enable the exploration of potential applications for the different fractions [39]. Mølgaard et al., determined the antimicrobial properties of 40 plant species used traditionally by the Huilliche people of Chile, among these T. corymbosus. Using a thin-layer chromatographic (TLC) agar overlay protocol, they determined a minimal inhibitory amount (MIA) against S. aureus (ATCC 6538) for a methanolic extract of T. corymbosus stem leaves, resulting in a value of ~1 mg [42].

3.4.3. Cytotoxic Properties

The study performed by Vidal-Pérez, evaluated the cytotoxic properties of several extracts of T. corymbosus using leaves and flowers from three different hosts: P. nigra, A. chilensis, and R. spinosus. They used extracts made with different solvents of increasing gradients of polarity. Results of the sulforhodamine B assay showed that the cell viability of AGS gastric cancer cell lines was significantly reduced by the highest concentration (50 μg/mL) of the ethyl acetate (~90% cell viability) and methanol (~70% cell viability) extracts of Tristerix flowers with P. nigra as a host. Similar concentrations of flower extracts with R. spinosus host prominently reduced cell viability at ~40% with ethyl acetate, and ~50% with methanol. Regarding the extracts of Tristerix with A. chilensis as host, the flower extracts at 50 μg/mL significantly reduced cell viability at ~50% with ethyl acetate as solvent and ~70% with methanol as solvent. Leaf extracts, in comparison, reduced cell viability of AGS to a lesser degree, with the best results (~50%) obtained from 50 μg/mL methanol extracts with A. chilensis as a host. The cytotoxic activity against PC-3 prostatic cancer cell lines was also evaluated, and the most significant results were observed on flower extracts. Extracts with R. spinosus as host in concentrations of 50 μg/mL resulted in a cell viability of ~50% with ethyl acetate, and ~60% with methanol, while flower extracts with A. chilensis as host resulted in a cell viability of ~70% with ethyl acetate as solvent. Concentrations of 100 μg/mL of the aforementioned extract resulted in a cell viability of ~40%. A final cytotoxicity assay was performed using MCF-7 breast cancer cells. Similar to the results obtained with PC-3 cells, the flower extract exhibited the highest cytotoxic activity. Ethyl acetate extracts with R. spinosus as host gave a cell viability of ~70% at concentrations of 50 μg/mL and ~40% at 100 μg/mL. Interestingly, dichloromethane extracts of leaves with the same host managed a significant reduction in cell viability, with a value of ~70% at its highest concentration, 50 μg/mL. A similar result was observed on these cell lines with extracts of flowers and leaves with A. chilensis as host, with the highest activity obtained from 100 μg/mL of ethyl acetate flower extracts (~50%) and 50 μg/mL of dichloromethane leaf extracts (~70%) [43].
Another work performed by Anicama-Lizarzaburo also studied the biological properties of T. chodatianus, focusing on its cytotoxic activities. An in vivo toxicity assay using Artemia salina revealed that the ethanolic extracts of leaves did not cause death in the animal models at any concentration tested, including the highest concentration of 1000 ppm, which had a survival rate of 96.7%. The same results were obtained in another toxicity assay using Lactuca sativa (Asteraceae) seeds, with no significant germinative reduction observed [44].

3.4.4. Analgesic Properties

In the work of Anicama-Lizarzaburo, analgesic properties of T. chodatianus extracts were also evaluated using a hot-plate test in a murine animal model. Testing of the analgesic effect was performed by orally administering to different animal groups various dilutions of leaf extract, saline solution as negative control, and tramadol as positive control, leaving them after 30 min of the treatment on the hot plate at 53.5 °C for a maximum of 30 s. It was observed that the negative control only lasted for a maximum of 8 s before showing an analgesic effect (paw licking or jumping out of the hot plate). Meanwhile, tests with dilutions of 400 mg/kg of leaf extracts showed an analgesic percentage of 95.19%, reflected by the longer duration of time of the animal models on the hot plate (longest time recorded of 18.10 s). Interestingly, concentrations of 200 and 600 mg/kg showed lower percentages of analgesia; 49.48% and 42.60%, respectively. In comparison with the positive control, tramadol resulted in an analgesia percentage of 165% (longest time recorded of 25.88 s). This confirms that, despite not being superior to the positive control, extracts of T. chodatianus possess significant analgesic properties [44].
Overall, the available evidence indicates that Tristerix spp. possess a broad spectrum of biological properties, including antioxidant, antimicrobial, cytotoxic, and analgesic activities, primarily attributed to their diverse phytochemical compositions. However, the magnitude of these effects varies according to the species, host plant, plant organ, extraction method, and experimental model employed. Despite these promising findings, the current evidence is largely limited to in vitro and preclinical studies. A summary of these results is shown in Table 3.
In this review, we explored the bioactive properties of Tristerix and their phytochemicals. Most of the studies found for this review discuss the presence of phenolic compounds and alkaloids. However, no study has directly tackled the presence of other secondary metabolites, such as volatile compounds or essential oils. There is speculation regarding the acquisition of volatile compounds from their hosts, but there is no study that has yet corroborated that theory [45]. The aforementioned compounds that had been found on Tristerix species have well-documented bioactive properties. Quercetin, one of its flavonoids, is found in several botanical sources, including some common fruits, vegetables, and medicinal plants. This compound has proven to exert anti-inflammatory and immunomodulatory activities based on different in vitro assays performed on animal and human cells, as well as in vivo assays on murine models. Most of the mechanisms involved are the inhibition of inflammatory intermediaries like interleukins (IL) IL-1β, IL-6, IL-8, tumor necrosis factor α (TNF-α), and enzymes such as cyclooxygenase (COX), among others [46]. Malvidin is another flavonoid, a member of the anthocyanin group, that possesses antioxidant and anti-inflammatory properties. As an antioxidant, it is capable of neutralizing free radicals by donating either an electron or a hydrogen atom and is capable of increasing the activity of antioxidant enzymes like catalase and superoxide dismutase. Meanwhile, the anti-inflammatory activities are associated with the modulation of pro-inflammatory cytokines and the inhibition of the NF-κB signaling pathway, which is related to the inflammatory response [47].
Apigenin is another flavonoid with a wide distribution on plant species and with well-studied bioactive properties. Various in vitro and in vivo studies have established its medicinal potential based on its antioxidant, anti-inflammatory, anti-tumoral, antidiabetic, and neuroprotective properties. Most of its activities are related to its inhibitory involvement with biological pathways related to inflammation and cell proliferation, as well as the neutralization of reactive oxidative species and stimulation of antioxidative enzymes such as glutathione and superoxide dismutase. The inhibition of certain enzymes, such as iNOS, COX-2, and MAO, is also related to the aforementioned biological activities. Neuroprotective activities are mainly associated with a reduction in fibrillar amyloid deposits and regulation of secretion of neurotransmitters such as GABA, serotonin, and dopamine, among others [1]. Catechin, another secondary metabolite found in Tristerix, shares some similar bioactive properties with apigenin, alongside cardioprotective, hepatoprotective, and nephroprotective activity, mainly related to its antioxidant nature [48].
Gallic acid is a phenolic acid that possesses a remarkable free radical scavenging capacity, widely used in the food industry as a flavoring agent and preservative. It is also known for its antimicrobial, anti-inflammatory, gastroprotective, cardioprotective, neuroprotective, and anti-tumoral properties. It was found that gallic acid can disrupt the integrity of the cell membrane on both Gram-positive and Gram-negative bacteria and can interfere with bacterial growth via inhibition of the dihydrofolate reductase. Gallic acid exerts most of its bioactive properties thanks to its antioxidant power, which in the case of its anti-tumoral properties can reduce carcinogenesis induced by reactive oxidative species through the increased activity of antioxidative enzymes. This phenolic acid also inhibits hyperglycemia and hypertriglyceridemia by increasing the cellular glucose uptake through stimulation of the PI3K/p-Akt signaling pathway, translocation of insulin-stimulated glucose transporters, and by reduction of the size of adipocytes [49].
Caffeic acid is a phenolic compound widely distributed in plant species, as well as one of the main components on propolis, and it also possesses antioxidant, anti-tumoral, and antibacterial properties [50]. Regarding the latter, its antibacterial effects are associated with its interaction with the cell membrane, leading to altered permeability and the inactivation of essential enzymes involved in energy production and structural synthesis. These antibacterial activities were assessed against bacteria such as S. aureus, E. coli, B. cereus, and L. monocytogenes, among others [51].
Luteolin, a flavonoid extracted from various species of the genus, has been studied due to its notable anti-inflammatory, anti-tumoral, and antioxidant properties. Research has demonstrated its capacity to inhibit cytokine production and signal transduction pathways, along with its ability to neutralize reactive oxygen species (ROS), indicating a promising therapeutic application in cancer prevention and treatment [52]. Rutin, another bioactive flavonoid extracted from T. tetrandus, has shown significant protection against oxidative stress as well as neuroprotective effects. These findings suggest its potential in the prevention of neurodegenerative diseases and in the modulation of the inflammatory response [53].
There is a key gap in the Tristerix phytochemical research. Currently, there are no studies on the seasonal variation of the phytochemical profile in Tristerix species. Additionally, there are no studies addressing the impact of environmental factors such as light and water and nutrient availability on the secondary metabolites of these mistletoe species. These factors (time of the year and environment) can greatly influence metabolic profile, both quantitatively and qualitatively [54,55,56]. However, since Tristerix species are parasitic, the impact of season and environmental factors is indirect, mainly via their effect on their hosts. Thus, the impact on their phytochemical profile may not be simply predicted as in non-parasitic species. This opens a relevant area for further phytochemical studies on Chilean Tristerix species, which could disentangle the possible direct and indirect effects of season and key environmental factors.

4. Patent Data

The patent search identified very little intellectual property activity regarding T. aphyllus, T. corymbosus, and T. verticillatus. The search effort undertaken in this review yielded no patent applications or patents granted for any phytochemicals, standardized extracts, extraction techniques, pharmaceutical preparations, nutraceutical products, or cosmetics based on these three species. The results only pertain to the species dealt with in this review and do not preclude patents for any other species of Tristerix or other mistletoe genus.

5. Conclusions

In summary, species from the Tristerix genus possess several bioactive compounds, such as phenolic acids, flavonoids, and anthocyanins, which are associated with antioxidant, anti-inflammatory, antimicrobial, and anti-tumoral properties. This information correlates with what is traditionally known about this hemiparasitic plant species and its use in ancestral cultures. Based on the presence of these phytochemicals, as well as the few studies performed on plant samples, it is clear that Tristerix species possess medicinal properties. Despite the results obtained in this review, there is a clear lack of quantitative correlation between the phytochemical content and pharmacological properties, meaning that further study is required to fully validate its pharmaceutical potential. Future research needs to focus on experimental assays, either in vitro or in vivo studios, before going into clinical trials in order to determine the mechanisms involved in their biological activity and the beneficial effects of this overlooked mistletoe. Future research should prioritize the quantitative characterization of bioactive metabolites, the establishment of composition–activity relationships, the elucidation of molecular mechanisms of action, comprehensive toxicological assessments, and well-designed preclinical and clinical studies. Such efforts will be essential to validate the therapeutic potential of Tristerix spp. and facilitate their translation into innovative pharmaceutical, nutraceutical, and biotechnological applications.

Author Contributions

Writing—Review and Editing: E.P.-S., C.A., G.G., D.V.-I., S.D.-C. and C.F.; M.R.-D., F.G.-F. and M.C.O. All authors have read and agreed to the published version of the manuscript.

Funding

This research received no external funding.

Data Availability Statement

No new data were created or analyzed in this study. Data sharing is not applicable to this article.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Salehi, B.; Sharifi-Rad, J.; Herrera-Bravo, J.; Salazar, L.A.; Delporte, C.; Barra, G.V.; Cazar Ramirez, M.-E.; López, M.D.; Ramírez Alarcón, K.; Martins, N.; et al. Ethnopharmacology, phytochemistry and biological activities of native Chilean plants. Curr. Pharm. Des. 2020, 26, 953–970. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  2. Otero, C.; Klagges, C.; Morales, B.; Sotomayor, P.; Escobar, J.; Fuentes, J.A.; Moreno, A.A.; Llancalahuen, F.M.; Arratia-Perez, R.; Gordillo-Fuenzalida, F.; et al. Anti-Inflammatory Chilean endemic plants. Pharmaceutics 2023, 15, 897. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  3. Scherson, R.A.; Albornoz, A.A.; Moreira-Muñoz, A.S.; Urbina-Casanova, R. Endemicity and evolutionary value: A study of Chilean endemic vascular plant genera. Ecol. Evol. 2014, 4, 806–816. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  4. Moreira-Muñoz, A. Plant Geography of Chile; Springer: Dordrecht, The Netherlands, 2011; p. 366. [Google Scholar]
  5. Díaz-Forestier, J.; León-Lobos, P.; Marticorena, A.; Celis-Diez, J.L.; Giovannini, P. Native useful plants of Chile: A review and use patterns. Econ. Bot. 2019, 73, 112–126. [Google Scholar] [CrossRef] [Scilit]
  6. Kuijt, J.; Hansen, B. Flowering Plants. Eudicots: Santalales, Balanophorale; The Families and Genera of Vascular Plants; Springer: Cham, Switzerland, 2015; Volume 12, pp. 1–213. [Google Scholar]
  7. Kuijt, J. Revision of Tristerix (Loranthaceae); Systematic Botany Monographs; American Society of Plant Taxonomists: Laramie, WY, USA, 1988; Volume 19, p. 1. [Google Scholar]
  8. Barlow-Canberra, B. Loranthaceae. Flora Malesiana; Series 1, Spermatophyta; National Herbarium of The Netherlands: Leiden, The Netherlands, 1997; Volume 13, pp. 209–401. [Google Scholar]
  9. Marticorena, A.; Alarcón, D.; Abello, L.; Atala, C. Plantas Trepadoras, Epífitas y Parásitas Nativas de Chile: Guía de Campo; CORMA: Mumba, India, 2010; ISBN 9789568398040. [Google Scholar]
  10. Rodríguez, R.; Marticorena, C.; Alarcón, D.; Baeza, C.; Cavieres, L.; Finot, V.L.; Fuentes, N.; Kiessling, A.; Mihoc, M.; Pauchard, A.; et al. Catálogo de las plantas vasculares de Chile. Gayana Botán. 2018, 75, 1–430. [Google Scholar] [CrossRef] [Scilit]
  11. Amico, G.C.; Rodriguez-Cabal, M.A.; Aizen, M.A. Geographic variation in fruit colour is associated with contrasting seed disperser assemblages in a south-Andean mistletoe. Ecography 2011, 34, 318–326. [Google Scholar]
  12. Cordero, S.; Gálvez, F.; Abello, L. Usos Tradicionales de la Flora de Chile. Volumen I, Nativas; Ediciones Botánicas, Editorial Planeta de Papel Ltd.a.: Valparaíso, Chile, 2020. [Google Scholar]
  13. Chateauneuf, R.; Benavides, M. Plantas Medicinales y Medicina Natural; Ocho Libros: Santiago, Chile, 2015; pp. 41–54. [Google Scholar]
  14. Hoffmann, A.; Arroyo, M.K.; Liberona, F.; Muñoz, M.; Watson, J. Plantas Altoandinas en la Flora Silvestre de Chile; Ediciones Fundación Claudio Gay: Santiago, Chile, 1998. [Google Scholar]
  15. Burgos, A.N.; Morales, M.A. Qualitative study of use medicinal plants in a complementary or alternative way with the use of among of rural population of the Bulnes city, Bío-Bío Region. Bol. Latinoam. Caribe Plantas Med. Aromat. 2010, 9, 377–387. [Google Scholar]
  16. Montenegro, G. Nuestra Flora Útil: Guía de Plantas de Uso Apícola, en Medicina Folklórica, Artesanal y Ornamental; Fundación Claudio Gay: Santiago, Chile, 2002; p. 267. [Google Scholar]
  17. Amico, G.C.; Vidal-Russell, R.; Nickrent, D.L. Phylogenetic relationships and ecological speciation in the mistletoe Tristerix (Loranthaceae): The influence of pollinators, dispersers, and hosts. Am. J. Bot. 2007, 94, 558–567. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Nicoletti, M. The anti-inflammatory activity of Viscum album. Plants 2023, 12, 1460. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  19. Kleszken, E.; Timar, A.V.; Memete, A.R.; Miere, F.; Vicas, S.I. On overview of bioactive compounds, biological and pharmacological effects of mistletoe (Viscum album L). Pharmacophore 2022, 13, 10–26. [Google Scholar] [CrossRef] [Scilit]
  20. Amico, G.C.; Nickrent, D.L. population structure and phylogeography of the mistletoes Tristerix corymbosus and T. aphyllus (Loranthaceae) using chloroplast DNA sequence variation. Am. J. Bot. 2009, 96, 1571–1580. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  21. Troncoso, A.J.; Cabezas, N.J.; Faúndez, E.H.; Urzúa, A.; Niemeyer, H.M. Host-mediated volatile polymorphism in a parasitic plant influences its attractiveness to pollinators. Oecologia 2009, 162, 413–425. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  22. Lucero, F.; Botto-Mahan, C.; Medel, R.; Fontúrbel, F.E. Nuevas evidencias sobre el muérdago Tristerix aphyllus (Loranthaceae): Interacción con especies frugívoras diurnas y nocturnas. Gayana Bot. 2014, 71, 270–272. [Google Scholar] [CrossRef] [Scilit]
  23. Del Rio, C.M.; Hourdequin, M.; Silva, A.; Medel, R. The influence of cactus size and previous infection on bird deposition of mistletoe seeds. Austral Ecol. 1995, 20, 571–576. [Google Scholar] [CrossRef] [Scilit]
  24. Medel, R. Assessment of parasite-mediated selection in a host-parasite system in plants. Ecology 2000, 81, 1554. [Google Scholar] [CrossRef] [Scilit]
  25. Silva, A.; del Rio, C.M.; del Rio, C.M. Effects of the mistletoe Tristerix aphyllus (Loranthaceae) on the reproduction of its cactus host Echinopsis chilensis. Oikos 1996, 75, 437. [Google Scholar] [CrossRef] [Scilit]
  26. Medel, R.; Botto-Mahan, C.; Smith-Ramírez, C.; Méndez, M.A.; Ossa, C.G.; Caputo, L.; Gonzáles, W.L. Historia natural cuantitativa de una relación parásito-hospedero: El sistema Tristerix-cactáceas en Chile semiárido. Rev. Chil. Hist. Nat. 2002, 75, 127–140. [Google Scholar] [CrossRef] [Scilit]
  27. Kraus, R.; Trimborn, P.; Ziegler, H. Tristerix aphyllus, a holoparasitic Loranthacea. Naturwissenschaften 1995, 82, 150–151. [Google Scholar] [CrossRef] [Scilit]
  28. Ojeda, S.; Arancibia, M.; Gómez, F.; Sepúlveda, I.B.; Orellana, J.I.; Fontúrbel, F.E. Spatial aggregation patterns in four mistletoe species: Ecological and environmental determinants. Plant Biol. 2023, 25, 1186–1195. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  29. Hoffmann, A.J.; Fuentes, E.R.; Cortés, I.; Liberona, F.; Costa, V. Tristerix tetrandrus (Loranthaceae) and its host-plants in the Chilean matorral: Patterns and mechanisms. Oecologia 1986, 69, 202–206. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  30. Aizen, M.A. Breeding system of Tristerix corymbosus (Loranthaceae), a winter-flowering mistletoe from the southern Andes. Aust. J. Bot. 2005, 53, 357–361. [Google Scholar] [CrossRef] [Scilit]
  31. Fontúrbel, F.E.; Franco, M.; Rodríguez-Cabal, M.A.; Rivarola, M.D.; Amico, G.C. Ecological consistency across space: A synthesis of the ecological aspects of Dromiciops gliroides in Argentina and Chile. Naturwissenschaften 2012, 99, 873–881. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Fontúrbel, F.E.; Medel, R. Frugivore-mediated selection in a habitat transformation scenario. Sci. Rep. 2017, 7, 45371. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  33. Fontúrbel, F.E.; Bruford, M.W.; Salazar, D.A.; Cortés-Miranda, J.; Vega-Retter, C. The hidden costs of living in a transformed habitat: Ecological and evolutionary consequences in a tripartite mutualistic system with a keystone mistletoe. Sci. Total Environ. 2019, 651, 2740–2748. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Fajardo, A.; Reyes-Bahamonde, C.; Fontúrbel, F.E.; Piper, F.I.; Callaway, R.M. Shining a new light on parasitic plants: Resistance to invasion. New Phytol. 2025, 247, 470–476. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  35. Piwowarczyk, R.; Ochmian, I.; Lachowicz, S.; Kapusta, I.; Sotek, Z.; Błaszak, M. Phytochemical parasite-host relations and interactions: A Cistanche armena case study. Sci. Total Environ. 2020, 716, 137071. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  36. Simirgiotis, M.J.; Quispe, C.; Areche, C.; Sepúlveda, B. Phenolic compounds in Chilean mistletoe (quintral, Tristerix tetrandus) analyzed by UHPLC–Q/Orbitrap/MS/MS and its antioxidant properties. Molecules 2016, 21, 245. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  37. Torres, P.; Saldaña, C.; Ortega, R.; González, C.; Torres, P.; Saldaña, C.; Ortega, R.; González, C. Determination of reducing power and phytochemical profile of the Chilean mistletoe “quintral” (Tristerix corymbosus (L) kuijt) hosted in “maqui” (Aristotelia chilensis), “huayún” (Rhaphitamnus spinosus) and “poplar” (Populus nigra). J. Chil. Chem. Soc. 2019, 64, 4645–4650. [Google Scholar] [CrossRef] [Scilit]
  38. Cifuentes-Araya, N.; Simirgiotis, M.; Sepúlveda, B.; Areche, C. Green separation by using nanofiltration of Tristerix tetrandus fruits and identification of its bioactive molecules through MS/MS Spectrometry. Plants 2024, 13, 1521. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. Velásquez, P.; Muñoz–Carvajal, E.; Luengo, M.; Bustos, D.; Galdames, F.; Gómez, M.; Montenegro, G.; Giordano, A. Phytochemical screening and biological properties of quintral flower polyphenolic fractions. Nat. Prod. Res. 2024, 40, 1612–1616. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  40. Alarcón-Acuña, J.D. Estudio Fitoquímico y Evaluación de la Actividad Antioxidante del Extracto Etanólico de Hojas de la Especie Tristerix chodatianus (Patschovsky) Kuijt “Pupa”; Universidad Nacional San Luis Gonzaga: Ica, Peru, 2021. [Google Scholar]
  41. Cabezas, N.J.; Urzúa, A.M.; Niemeyer, H.M. Translocation of isoquinoline alkaloids to the hemiparasite, Tristerix verticillatus from its host, Berberis montana. Biochem. Syst. Ecol. 2009, 37, 225–227. [Google Scholar] [CrossRef] [Scilit]
  42. Mølgaard, P.; Holler, J.G.; Asar, B.; Liberna, I.; Rosenbæk, L.B.; Jebjerg, C.P.; Jørgensen, L.; Lauritzen, J.; Guzman, A.; Adsersen, A.; et al. Antimicrobial evaluation of huilliche plant medicine used to treat wounds. J. Ethnopharmacol. 2011, 138, 219–227. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. Vidal-Pérez, D. Efectos del Quintral (Tristerix corymbosus) Extractos de Hoja y de Flor en la Viabilidad y Muerte Celular de Líneas Celulares de Cáncer de Mama, Próstata y Gástrico In Vitro. 2019. Available online: https://repositoriobibliotecas.uv.cl/serveruv/api/core/bitstreams/7956d1ec-66d2-4e63-b0cb-47b4ebc17be9/content (accessed on 7 March 2025).
  44. Anicama-Lizarzaburo, C.L. Evaluación de La Actividad Analgésica y Citotoxicidad del Extracto Etanólico de Hojas de la Especie Tristerix chodatianus (Patsch.) Kuijt “Pupa”; Universidad Nacional San Luis Gonzaga: Ica, Peru, 2022. [Google Scholar]
  45. Pincheira, J.; Villarroel, J.; Orellana, J.I.; Fontúrbel, F.E. A tale of two mistletoes: Phenology and fauna associated with two sympatric species. Botany 2024, 102, 98–107. [Google Scholar] [CrossRef] [Scilit]
  46. Li, Y.; Yao, J.; Han, C.; Yang, J.; Chaudhry, M.T.; Wang, S.; Liu, H.; Yin, Y. Quercetin, inflammation and immunity. Nutrients 2016, 8, 167. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  47. Merecz-Sadowska, A.; Sitarek, P.; Kowalczyk, T.; Zajdel, K.; Jęcek, M.; Nowak, P.; Zajdel, R. Food anthocyanins: Malvidin and its glycosides as promising antioxidant and anti-inflammatory agents with potential health benefits. Nutrients 2023, 15, 3016. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  48. Ganeshpurkar, A.; Saluja, A. The pharmacological potential of catechin. Indian J. Biochem. Biophys. 2020, 57, 505–511. [Google Scholar] [CrossRef] [Scilit]
  49. Kahkeshani, N.; Farzaei, F.; Fotouhi, M.; Alavi, S.S.; Bahramsoltani, R.; Naseri, R.; Momtaz, S.; Abbasabadi, Z.; Rahimi, R.; Farzaei, M.H.; et al. Pharmacological effects of gallic acid in health and diseases: A mechanistic review. Iran. J. Basic Med. Sci. 2019, 22, 225. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  50. Pavlíková, N. Caffeic acid and diseases-mechanisms of action. Int. J. Mol. Sci. 2022, 24, 588. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  51. Magnani, C.; Isaac, V.L.B.; Correa, M.A.; Salgado, H.R.N. Caffeic acid: A review of its potential use in medications and cosmetics. Anal. Methods 2014, 6, 3203–3210. [Google Scholar] [CrossRef] [Scilit]
  52. Maryam, S.; Khalid, S.; Arshad, A.; Abid, S.; Iqbal, L.Z.; Amjad, Y.; Faisal, S.; Maryam, S.; Khalid, S.; Arshad, A.; et al. luteolin: A versatile flavonoid for anti-inflammatory, anti-cancer, and neuroprotective therapies. GSC Biol. Pharm. Sci. 2024, 29, 119–137. [Google Scholar] [CrossRef] [Scilit]
  53. Iriti, M.; Varoni, E.M.; Vitalini, S. Bioactive compounds in health and disease—Focus on rutin. Bioact. Compd. Health Dis. 2023, 6, 235–242. [Google Scholar] [CrossRef] [Scilit]
  54. Ogwu, M.C.; Izah, S.C.; Joshua, M.T. Ecological and environmental determinants of phytochemical variability in forest trees. Phytochem. Rev. 2025, 24, 5109–5137. [Google Scholar] [CrossRef] [Scilit]
  55. Liebelt, D.J.; Jordan, J.T.; Doherty, C.J. Only a matter of time: The impact of daily and seasonal rhythms on phytochemicals. Phytochem. Rev. 2019, 18, 1409–1433. [Google Scholar] [CrossRef] [Scilit]
  56. Zamani, S.; Bakhshi, D.; Ebadi, M.T.; Sahraroo, A. Phytochemical profile and antioxidant activity of Dracocephalum kotschyi boiss. affected by environmental conditions of cultivation regions. BMC Plant Biol. 2025, 25, 968. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Tristerix corymbosus. (A) Leaves and flowers. (B) Leaves and fruits. Original photograph provided by the authors.
Scipharm 94 00066 g001
Figure 2. Dendogram using Neighbor-joining of ITS1 section of several Tristerix spp. Phylogenetic analysis was performed using ITS sequences from the genus Tristerix, such as T. aphyllus (DQ442964), T. corymbosus (DQ442969), T. verticillatus (DQ442974), T. chodatianus (DQ442976), T. peruvianus (DQ442977), T. grandiflorus (DQ442978), T. longebracteatus (DQ442981), and T. pubescens (DQ442984). As outgroup, a sequence of Rubus idaeus (AF055756) was used.
Scipharm 94 00066 g002
Figure 3. Chemical structures of the main phytochemicals identified in Tristerix spp. (A) Phenolic acids. (1) 3-O-caffeoylquinic acid, (2) 5-O-caffeoylquinic acid, (3) caffeic acid, (4) cryptochlorogenic acid, (5) gallic acid, (6) p-coumaric acid, and (7) sinapic acid (B) Flavonoids. (1) apigenin, (2) catechin, (3) luteolin, (4) malvidin, (5) naringenin, (6) quercetin, (7) quercetin-3-O-glucoside, and (8) rutin (C). Alkaloids. (1) pronuciferine and (2) glaucine.
Scipharm 94 00066 g003
Table 1. Hosts found to be infected by Tristerix spp. in Chile.
SpeciesNative HostsIntroduced HostReferences
T. aphyllusLeucostele spp. (Cactaceae), Eulychnia spp. (Cactaceae), rarely species of Copiapoa and Opuntia (Cactaceae)Not known[7,22,23,25,26,27]
T. corymbosusGevuina avellana (Proteaceae), Kageneckia oblonga (Rosaceae), Aristotelia chilensis (Elaeocarpaceae), Retanilla trinervia (Rhamnaceae), Azara integrifolia (Salicaceae), Peumus boldus (Monimiaceae), Rhaphithamnus spinosus (Verbenaceae), Berberis darwinii (Berberidaceae), Colletia hystrix (Rhamnaceae), Maytenus boaria (Celastraceae), Colliguaja odorifera (Euphorbiaceae) and Luma apiculata (Myrtaceae)Salix spp. (Salicaceae), Populus spp. (Salicaceae), Acacia dealbata and A. melanoxylon (Fabaceae)[7,11,28,29,30]
T. verticillatusEphedra andina (Ephedraceae), Schinus polygama (Anacardiaceae), Colletia hystrix (Rhamnaceae), Quillaja saponaria (Quillajaceae), Vachellia caven (Fabaceae), Escallonia illinita (Escalloniaceae) Luma apiculata (Myrtaceae) Discaria chacaye (Rhamnaceae), Schinus montanus (Anacardiaceae), Fabiana imbricata (Solanaceae) and Berberis montana (Berberidaceae)Not known[7,17,21,28]
Table 2. Summary of phytochemical studies on Tristerix species.
SpeciePlant OrganExtraction Solvent/MethodAnalytical TechniqueMajor Identified CompoundsCollection Site/HostReference
Tristerix tetrandusLeaves and flowersMethanolic extracts for antioxidant assaysUHPLC-PDA-HESI-Orbitrap MSChlorogenic acid, catechin, rutin, quercetin-3-O-glucoside, quercetin-3-O-pentose, 5-O-caffeoylquinic acid, cyanidin-3-glucoside, malvidin, quercetin, luteolin, naringenin, apigeninNot reported[36]
Tristerix corymbosusLeaves and flowersSequential extraction with hexane, dichloromethane, ethyl acetate and methanolQualitative phytochemical screeningTannins, flavonoids, steroids, quinones, saponins, triterpenes, cardiac glycosidesHosts: Populus nigra, Aristotelia chilensis, Rhaphithamnus spinosus (Chile)[37]
Tristerix tetrandusFruitsNanofiltration (polyamide-TFC NF membranes)UHPLC-ESI-MS/MSGallic acid, cryptochlorogenic acid, chlorogenic acid, caffeic acid, p-coumaric acid, rutin, quercetinNot reported[38]
Tristerix corymbosusFlowersFractionation into free, esterified and insoluble phenolic fractionsPhenolic profilingChlorogenic acid, p-coumaric acid, sinapic acidNot reported[39]
Tristerix chodatianusLeavesEthanolic extractionPhytochemical screeningPhenolic compounds, flavonoids, triterpenes, steroids, leucoanthocyanidins, saponinsPolylepis spp., Peru[40]
Tristerix verticillatusLeavesAlkaloid extractionAlkaloid analysis/comparative phytochemical analysisPronuciferine, glaucineHost comparison: Berberis montana vs. Schinus montanus[41]
Table 3. Summary of the biological properties reported for Tristerix spp. extracts.
SpeciePlant OrganExtract/FractionExperimental ModelBiological ActivityMain FindingsReference
T. tetrandusLeaves and flowersMethanolic extractsDPPH, FRAPAntioxidantLeaves showed higher DPPH radical scavenging activity, whereas flowers exhibited greater FRAP reducing power associated with higher anthocyanin content.[36]
T. corymbosusLeaves and flowers from different hostsMethanol, ethyl acetate and other solvents Reducing power assay Antioxidant Antioxidant capacity varied according to host species, plant organ, and extraction solvent, reflecting differences in secondary metabolite composition [37]
T. corymbosusDifferent fractionsFree, esterified and insoluble fractionsDPPH, ABTS, FRAPAntioxidantAll fractions exhibited antioxidant activity, with variations depending on phenolic composition.[39]
T. chodatianusLeavesEthanolic extractDPPH, FRAPAntioxidantDose-dependent antioxidant activity (DPPH IC50 = 0.242 mg/mL; FRAP TEAC = 0.642 ± 0.008 mg/mL).[40]
T. corymbosusDifferent fractionsFree and esterified fractionsE. coli, S. enterica serovar Typhi, S. aureusAntimicrobialAntibacterial activity correlated with chlorogenic, sinapic and p-coumaric acids.[39]
T. corymbosusStem leavesMethanolic extractS. aureus (TLC agar overlay)AntimicrobialMinimal inhibitory amount of approximately 1 mg.[42]
T. corymbosusLeaves and flowers from different hostsDichloromethane, ethyl acetate, methanolAGS, PC-3, MCF-7 cell linesCytotoxicFlower extracts showed stronger cytotoxicity than leaf extracts. Activity depended on host species, extraction solvent, and cancer cell line.[43]
T. chodatianusLeavesEthanolic extractArtemia salina and Lactuca sativaCytotoxicNo significant toxicity under evaluated conditions.[44]
T. chodatianusLeavesEthanolic extractHot-plate test (mice)AnalgesicSignificant analgesic effect, greatest response at 400 mg/kg.[44]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.