
Article

Conservation and Targeted Wild Tending of Schisandra chinensis Under Global Change: Informed by SDMs and Fingerprint Analysis of Climate–Land–Composition Responses

Heilongjiang Research Center of Genuine Wild Medicinal Materials Germplasm Resources, School of Life Sciences and Technology, Harbin Normal University, Harbin 150025, China
*
Authors to whom correspondence should be addressed.
These authors contributed equally to this work.
Biology 2026, 15(17), 1501; https://doi.org/10.3390/biology15171501
Submission received: 22 July 2026 / Revised: 19 August 2026 / Accepted: 25 August 2026 / Published: 2 September 2026

Simple Summary

Schisandra chinensis (Turcz.) Baill. is a valuable medicinal plant resource, and the demand for its wild resources has been continuously increasing in recent years. However, the response mechanism of its future habitat suitability and medicinal quality to global change remains poorly understood. This study comprehensively evaluated the suitable habitats, spatial distribution of medicinal quality, and conservation priority of S. chinensis by integrating future climate scenario simulation, dynamic prediction of land use, and high-performance liquid chromatography (HPLC) fingerprint data. The results showed that within the planned S. chinensis protected areas in Heilongjiang Province, the area actually covered by existing nature reserves only accounts for 4.281%, and significant conservation gaps exist in the Greater Khingan Range and Laoye Range. Based on the spatial distribution trend of the chemical component content of S. chinensis under future climate change, it is recommended that priority wild tending measures be implemented in Tahe County and Huma County in the Greater Khingan Range region. This study can provide a scientific basis for the conservation and targeted wild tending of S. chinensis.

Abstract

Schisandra chinensis (Turcz.) Baill. is a valuable medicinal plant species, and the demand for its wild resources is increasing continuously. However, the response mechanisms of its future habitat suitability and medicinal quality to global change remain poorly understood. This study integrated future climate projections under multiple Shared Socioeconomic Pathway (SSP) scenarios, land use dynamics, high-performance liquid chromatography (HPLC) fingerprint data, and an ensemble species distribution model to assess the habitat suitability, medicinal quality and conservation priorities of S. chinensis. Model performance evaluation indicated that the Biomod2 ensemble model achieves high prediction accuracy, with a True Skill Statistic (TSS) value of 0.882. Under the combined threat of climate change and land use change, the area of suitable habitat for S. chinensis in Heilongjiang Province will only account for 20.471% of the current suitable habitat area under the SSP5-8.5 scenario in the 2090s, and most suitable habitats will shift to the Greater Khingan Range region. The responses of different medicinal components of S. chinensis to future climate change vary considerably: for instance, the area of high-quality distribution for Schisandrol A and Gomisin A shows an overall expanding trend compared with the current status under future climate scenarios, while the area of high-quality distribution for Schizandrin B shows an overall shrinking trend. Within the planned conservation area for S. chinensis in Heilongjiang Province, the coverage of existing nature reserves is only 4.281%, and obvious conservation gaps exist in the Greater Khingan Range and Laoye Mountains regions. In response to the spatial distribution characteristics of the medicinal component content of S. chinensis under future climate change, we recommend implementing wild tending of S. chinensis in Tahe County and Huma County of the Greater Khingan Range region. The above findings provide a theoretical basis for the conservation and wild tending of S. chinensis.

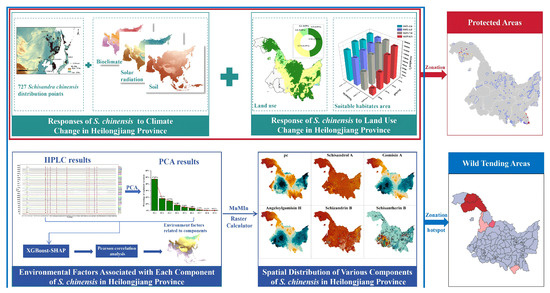
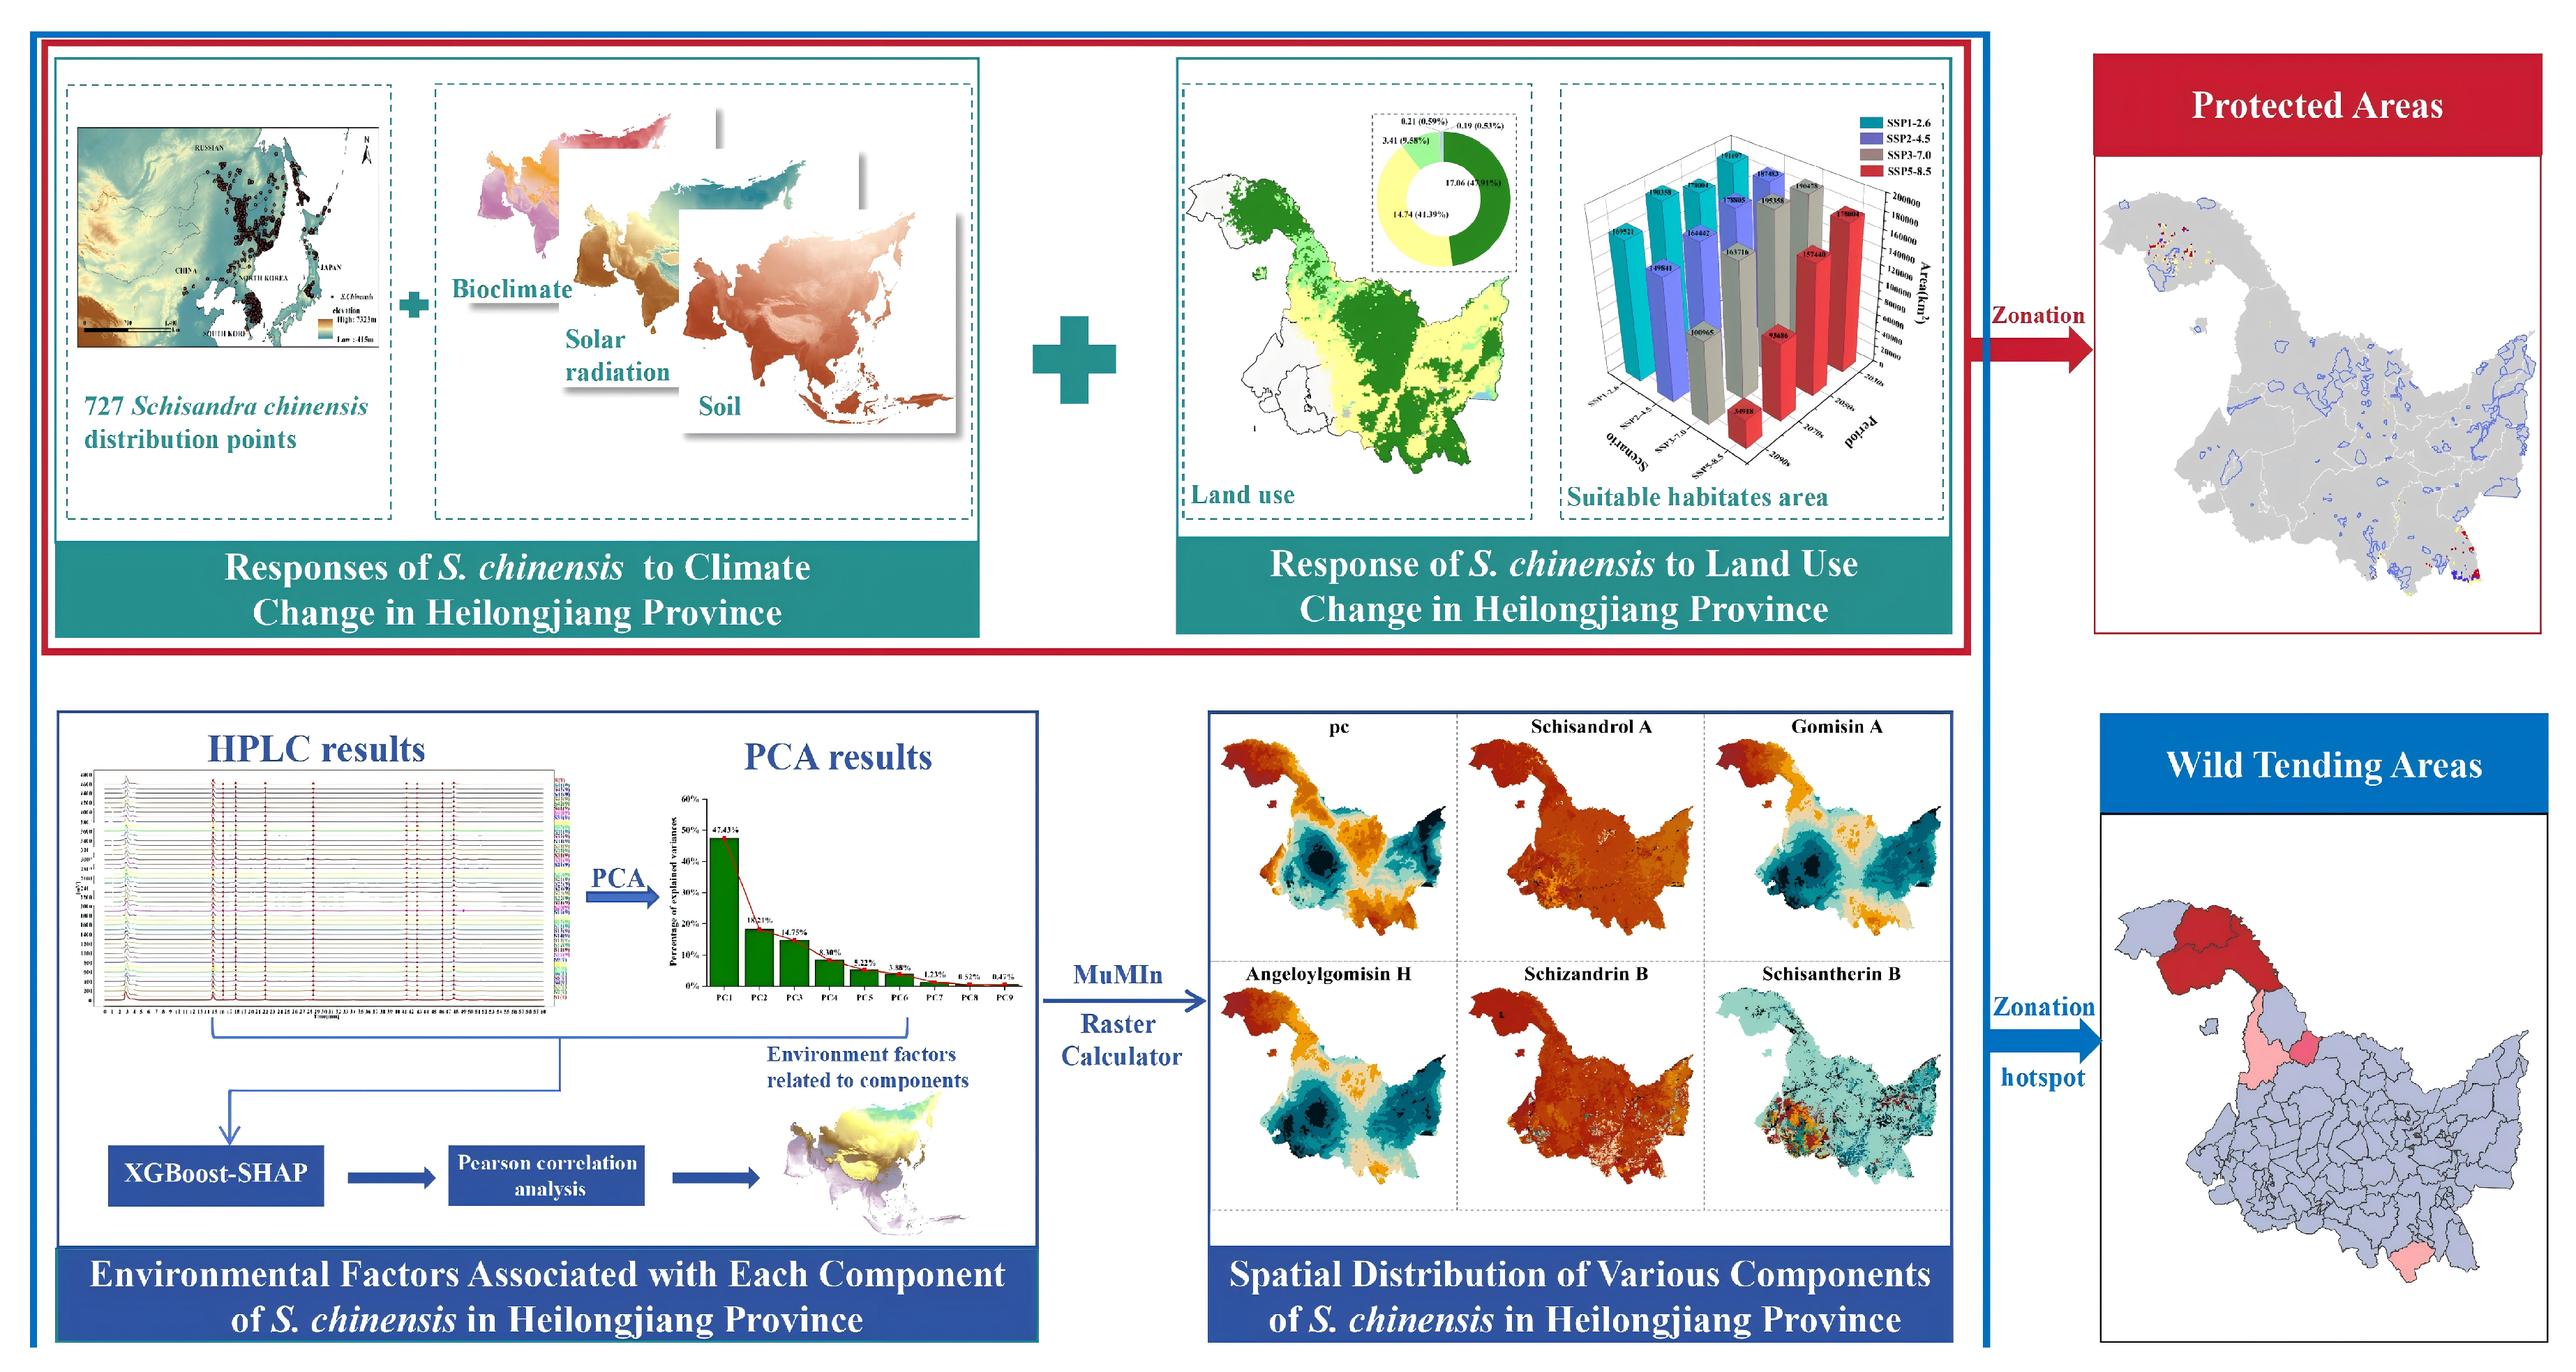
Graphical Abstract

1. Introduction

For thousands of years, plants have been the faithful partners on which humankind relies for survival, providing us with staple food to sustain ourselves and safeguarding our well-being [1]. It is estimated that 70% to 80% of the global population primarily relies on traditional herbal medicine to meet its basic healthcare needs [2]. As the population continues to grow and access to Western medicine (i.e., symptomatic treatment) remains generally limited in developing countries, demand for medicinal plants will continue to rise [3]. Some studies indicate that 70–90% of medicinal and aromatic plants are wild-harvested [4]. The growing demand for medicinal plants has placed enormous pressure on wild medicinal plant populations, and numerous species are currently at risk of extinction due to excessive overharvesting in wild habitats [5]. Therefore, it is crucial to protect the wild resources of medicinal plants and maintain a balance between their availability and medical demand. Currently, academia has proposed multiple strategies to address the shortage of wild medicinal plant resources, including in situ conservation (e.g., nature reserves and wild nurseries), ex situ conservation (e.g., botanical gardens and seed banks), and commercial cultivation [6,7,8,9]. Long-term production practices demonstrate that under the influence of specific ecological environments and anthropogenic factors, medicinal plants exhibit distinct regional characteristics [10,11]. Wild tending of Chinese medicinal materials, which relies on the natural habitats of medicinal plants supplemented with moderate human intervention, aims to maximize the restoration of the wild traits of medicinal materials. This approach effectively alleviates the contradiction between the shortage of wild resource supply and the continuous growth of market demand, and ensures the production of Chinese medicinal materials with authenticity and superior quality [12]. Accordingly, it is urgent to systematically elucidate the multi-scale interaction network between wild medicinal plants and various environmental factors, conduct in-depth analysis of their geospatial distribution patterns, and thereby provide an accurate theoretical framework for the scientific conservation and sustainable utilization of wild medicinal plant populations.
Climate change has been an inherent part of Earth’s evolutionary history and will continue to affect all aspects of plants in the future [13,14]. Furthermore, with the intensification of anthropogenic activities, climate change has become increasingly pronounced, and extreme weather events have also grown more frequent [15]. Driven by ongoing global climate change, biodiversity is experiencing an unprecedented decline this century [16]. Research findings indicate that climate change is projected to alter plant distribution patterns: species will expand into newly suitable habitats while declining in increasingly stressful environments [17]. Against this backdrop, how the distribution pattern of medicinal plants responds to climate change has become a key theoretical basis. It underpins the scientific conservation of their wild resources and the rational planning of planting layouts. Furthermore, the regional dependence of high-quality medicinal materials renders them particularly sensitive to climate change. Climate-driven distribution range migration not only threatens the survival of existing high-quality planting areas, but is also directly manifested as yield loss and quality alteration, which are the most intuitive signals of climate shocks. Most existing studies generally regard climate change as the sole dominant factor affecting biodiversity, while ignoring the key variable of land use change, and even fail to address the superposition effect generated by the interaction between the two factors [18]. Land use change may not only cause the loss of species habitats, but also trigger cascading effects such as the fragmentation of remaining habitats and the increase in agrochemical input into surrounding natural (or semi-natural) habitats [19,20]. Therefore, by incorporating global climate change and land use change into a unified analytical framework, we can achieve a more comprehensive assessment of the current and future potential distribution dynamics of medicinal plant populations. This approach can provide scientific knowledge support for reconciling the relationship between the conservation of wild medicinal plant resources and the demand for medicinal healthcare.
Schisandra chinensis (Turcz.) Baill. is a woody vine species belonging to the genus Schisandra of the family Schisandraceae. Its populations are mainly distributed in Northeast Asia, with the temperate forest vegetation region of China as its core distribution area [21]. S. chinensis Fructus is used as a medicine in the form of its dried ripe fruit. It exhibits the therapeutic effects of astringent and consolidating, enhancing qi while nourishing fluid, and tonifying the kidney and calming the mind. It demonstrates remarkable efficacy in the treatment of persistent cough with dyspnea due to deficiency, nocturnal emission and spermatorrhea, enuresis and frequent urination, persistent chronic diarrhea, spontaneous sweating and night sweating, impaired fluid with thirst due to yin deficiency, internal heat-induced consumptive thirst, palpitations and insomnia [22]. In natural habitats, S. chinensis seeds exhibit innate dormancy. The germination rate remains at a low level even after cold stratification treatment. This results in difficulties in sexual propagation of this species [23]. In addition, the differentiation ratio of female flowers is highly sensitive to changes in light conditions, and its instability directly triggers the common alternate bearing cycle in actual production, which has become a key bottleneck restricting the stable fruit yield of S. chinensis [24]. Given that S. chinensis struggles to achieve large-scale propagation via seeds in its natural habitat, and its wild resources have been excessively consumed, S. chinensis is listed as a Class Three protected plant in the National List of Rare and Endangered Medicinal Animal and Plant Species [25]. With the accelerated decline of wild S. chinensis resources driven by anthropogenic destruction and global change, the imbalance between the conservation and supply of S. chinensis resources has become increasingly prominent. Several critical limitations currently exist in species distribution modeling studies of S. chinensis: First, climate change is generally regarded as the sole driving factor. However, land use change and its potential interactive effects with climate change have been completely neglected. Second, existing studies are only limited to predicting the shift in population distribution ranges. They also fail to incorporate the spatial distribution pattern of the content of pharmaceutically active ingredients (such as lignans) into the analytical framework. As a result, it is impossible to assess the impact of environmental changes on the quality of S. chinensis medicinal materials [26,27,28,29,30].
To address the aforementioned research gaps, this study integrates multi-source data including environmental conditions, land use patterns and chemical compositions. It then innovatively couples ensemble species distribution models (SDMs), phytochemical prediction and conservation priority ranking, and develops a multi-dimensional analytical framework for the conservation and targeted wild tending of S. chinensis in Heilongjiang Province. Based on the above analytical framework, this study sets three core objectives as follows: first, to deeply analyze the functional mechanism of dominant environmental factors in regulating the population dynamics of S. chinensis and the accumulation process of its bioactive chemical components; second, to systematically elucidate the response pattern of the spatial distribution pattern of S. chinensis populations and the quality of its medicinal materials to climate change; third, based on future climate change and land use scenarios, to comprehensively determine the optimal spatial allocation scheme for the conservation of wild S. chinensis resources and targeted wild tending in Heilongjiang Province.

2. Materials and Methods

2.1. Simulation of Current and Future Suitable Habitats for S. chinensis

2.1.1. Acquisition of Species Distribution Points and Collection of Medicinal Materials of S. chinensis

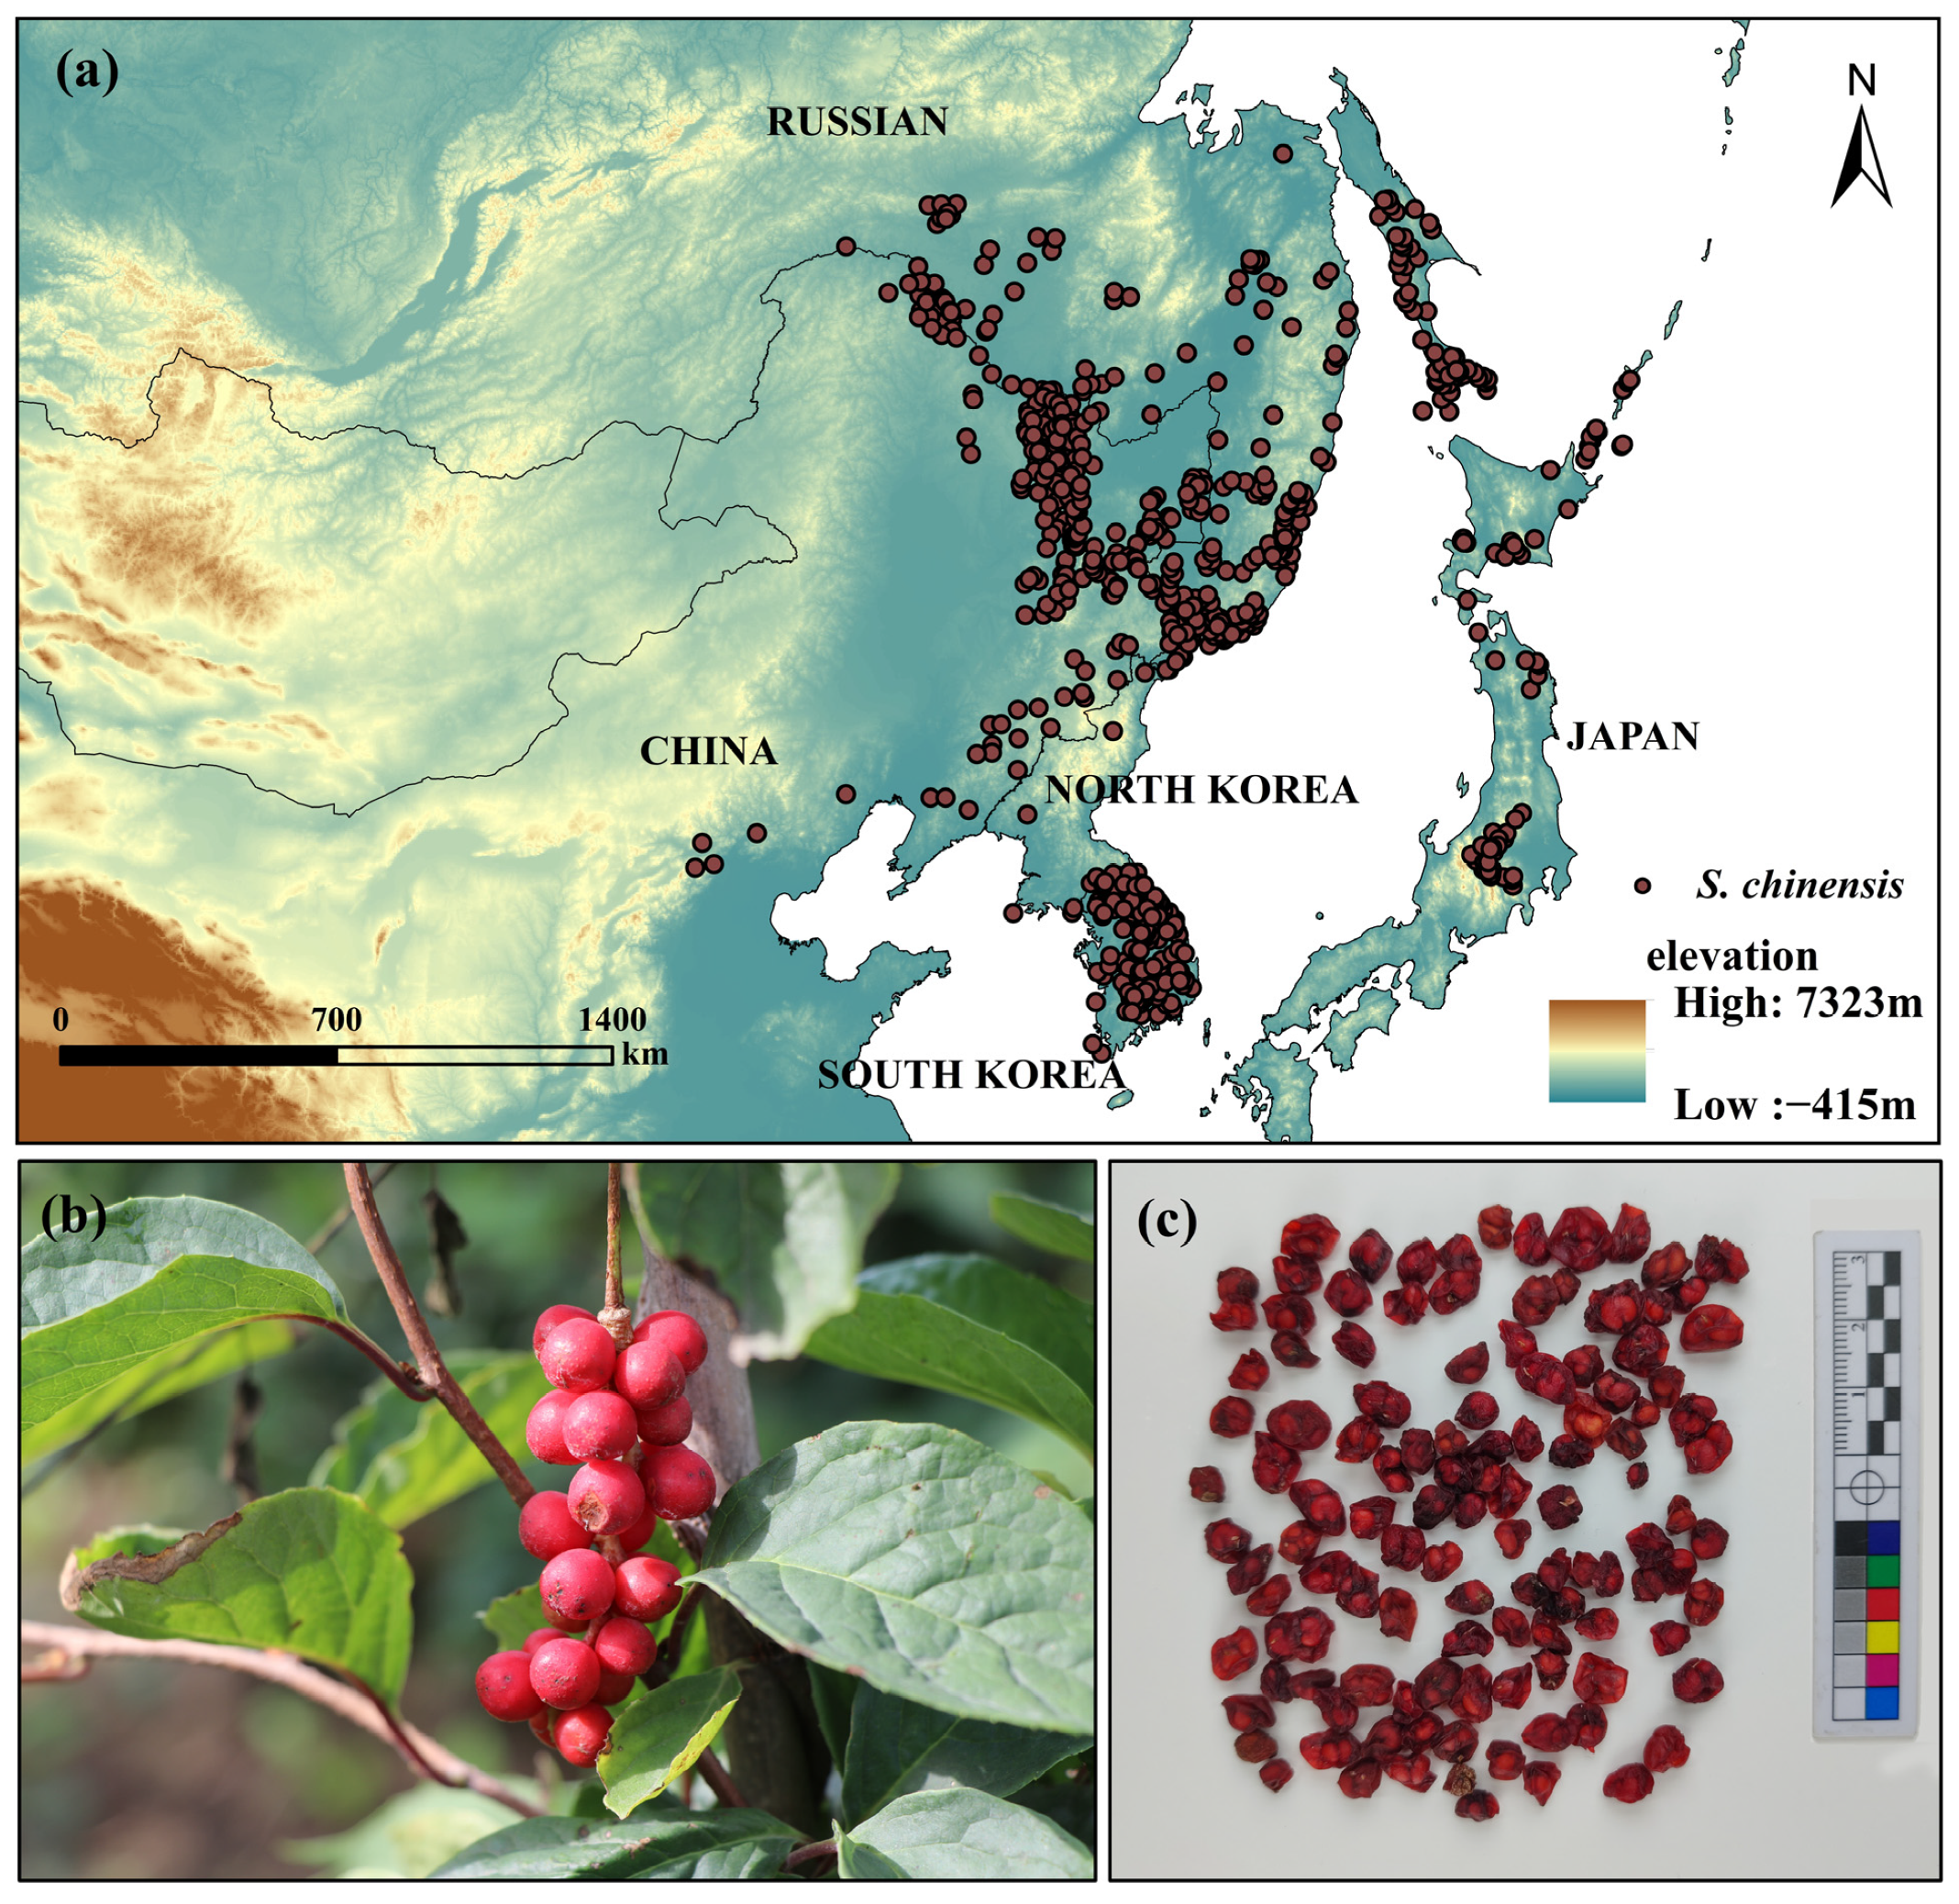
A total of 2131 occurrence records of S. chinensis from 2000 to the present were obtained through field surveys across Heilongjiang Province and global data retrieval from multiple online platforms, including the National Specimen Information Infrastructure (http://www.nsii.org.cn/, accessed on 20 September 2025), the Global Biodiversity Information Facility (GBIF.org, (https://doi.org/10.48580/dgykv, accessed on 20 September 2025)), and the Chinese Virtual Herbarium (http://www.cvh.ac.cn/, accessed on 20 September 2025). Given that species identification is fundamental to species conservation, we verified specimens sourced from global datasets, and eliminated records with erroneous identifications as well as those from non-suitable habitats, such as highways and residential areas [31]. Subsequently, we employed ENMtools to retain only one occurrence point within a 5 km grid. Finally, 727 occurrence points were retained for model construction (Figure 1). A total of 46 batches of S. chinensis medicinal materials (mature fruits of S. chinensis) were collected from various districts and counties in Heilongjiang Province. The collection was concentrated in the fructescence of S. chinensis fruits in each region. Specific collection time and sampling locations are shown in Supporting Information of The Chromatographic Fingerprint. After collection, impurities were removed and the materials were uniformly sun-dried. The identification of all the above data points was assisted and processed by Professor Wang Chen from Harbin Normal University.

2.1.2. Acquisition of Environmental Variables and Geographic Data

In species distribution modeling, factors closely associated with plant physiology and ecological responses should be prioritized to effectively guarantee the reliability of prediction results [32]. Accordingly, this study comprehensively considered the ecological characteristics of S. chinensis; that is, S. chinensis favors sunlight and moisture, and has specific requirements for temperature and soil conditions. A total of 35 environmental variables (including climate, solar radiation, and soil physical and chemical properties—see Table S1) were incorporated in this study to simulate the distribution range of this species [29,33,34]. Nineteen climatic factors from 2000 to 2018 (e.g., mean diurnal temperature range, temperature seasonality, precipitation of the driest quarter, etc.) were downloaded as climatic variables from the WorldClim database (v2.1) (www.worldclim.org, accessed on 20 September 2025). Solar radiation (Srad) data covering 1970–2000 was also obtained from the WorldClim database (v2.1), which was processed via the raster calculator in ArcMap 10.5 to generate solar radiation values for four seasons, to better align with the growth and development of S. chinensis. Since the root system of S. chinensis is distributed in shallow soil layers and its growth is affected by soil organic matter, pH and soil, 12 shallow soil variables including calcium carbonate or lime content (CaCO3) and pH of topsoil (0–30 cm) were downloaded from the Harmonized World Soil Database (HWSD). All environmental variables have a spatial resolution of 2.5 arc-minutes.
Subsequently, we incorporated these environmental variables and species distribution coordinates into the Maximum Entropy (MaxEnt) model, which can accurately identify important variables by generating a relative contribution table [35]. Based on Table S2, we discarded environmental variables with a contribution of less than 0. Next, we performed Pearson’s rank correlation analysis on the remaining environmental variables using the ENMtools v 1.0.4 software [36], and retained the environmental variables with high contribution and low correlation coefficients (r, |r| < 0.8), as shown in Table S3. Based on the Pearson correlation analysis, this study further calculated the variance inflation factor (VIF) of each environmental factor to eliminate the interference of potential multicollinearity among environmental factors on model estimation [37]. With VIF < 10 set as the tolerance threshold for multicollinearity, the results show that the VIF values of all factors range from 1.1 to 6.2 (see Table 1), which are far below the critical value. This indicates that there is no severe multicollinearity among the selected environmental factors, and all factors can be included simultaneously in subsequent analyses. Finally, 17 environmental variables were retained (Table 1).
To evaluate the impact of climate change on the potential suitable distribution area of S. chinensis and reduce prediction uncertainty caused by a single general circulation model, this study selected three widely adopted general circulation models (CNRM-CM6-1 (Centre National de Recherches Météorologiques—Climate Model Version 6), MIROC-ES2L (Model for Interdisciplinary Research on Climate, Earth System version 2 for Long-term simulations) and MRI-ESM2-0 (Meteorological Research Institute Earth System Model version 2.0)) from the WorldClim climate database, and applied their equally weighted averaged outputs to subsequent analyses. The selected models are commonly used in species distribution modeling and exhibit high applicability [38,39,40]. Each of the aforementioned general circulation models incorporates four Shared Socioeconomic Pathways (SSP1-2.6 (Shared Socioeconomic Pathway 1-2.6 (Sustainability)), SSP2-4.5 (Shared Socioeconomic Pathway 2-4.5 (Middle of the Road)), SSP3-7.0 (Shared Socioeconomic Pathway 3-7.0 (Regional Rivalry)) and SSP5-8.5 (Shared Socioeconomic Pathway 5-8.5 (Fossil-fueled Development))), and for each pathway, four time periods are extracted: 2021–2040 (2030s), 2041–2060 (2050s), 2061–2080 (2070s), and 2081–2100 (2090s). Due to the absence of available corresponding future data for solar radiation and soil properties, this study treats solar radiation and soil factors as static variables in species distribution modeling. The spatial resolution of all the aforementioned environmental variables is 2.5 arc-minutes.
To elucidate the potential impacts of land use change on the habitat suitability of S. chinensis, this study integrated land use data when constructing suitable habitat. The current (2020) land use data were obtained from the MODIS dataset provided by the National Aeronautics and Space Administration (NASA) Earth Data Platform (https://search.earthdata.nasa.gov/search/, accessed on 20 September 2025); the future land use data were sourced from the research findings of Hou et al. (https://doi.org/10.6084/m9.figshare.20088368.v1, accessed on 20 September 2025), and four sets of scenario data corresponding to different climate scenarios (SSP1-2.6, SSP2-4.5, SSP3-7.0, SSP5-8.5) were selected. All land use data were resampled to a resolution of 2.5 arc-minutes using ArcMap 10.5 software.
Maps of China’s administrative divisions and nature reserves were obtained from the National Geomatics Center of China (https://www.webmap.cn/, accessed on 20 September 2025). MaxEnt version 3.4.4 was downloaded from the following website: http://biodiversityinformatics.amnh.org/open_source/maxent/, accessed on 20 September 2025. This study employed ArcGIS 10.5 and RStudio 4.0.4 for data analysis and processing.

2.1.3. Simulation of Suitable Habitats for S. chinensis Under Current and Future Climate Scenarios

Biomod2 R Package (v3.5.1) in R 4.0.4 was used to simulate the potential suitable distribution areas of S. chinensis under climate change. Biomod2 is an integrated R package specifically designed for species distribution modeling, which supports multiple algorithms and their integrated ensembles [41]. In this study, ten modeling algorithms, namely GLM (General Linear Model), GBM (Gradient Boosting Machine), GAM (Generalized Additive Model), CTA (Classification and Regression Tree Analysis), ANN (Artificial Neural Network), SRE (Site Reliability Engineering), FD (Functional Data), MARS (Multivariate Adaptive Regression Splines), RF (Random Forest) and MaxEnt (Maximum Entropy Model), are employed and have been proven to have good predictive performance [41,42]. Research findings indicate that the prediction performance of the MaxEnt model is closely correlated with feature combination (FC) and regularization multiplier (RM). The MaxEnt model constructed with default parameters is prone to overfitting, which results in low transferability of the model, and the derived prediction results are not optimal and may even be unreliable [43,44]. Accordingly, we tuned the feature combination (FC) and regularization multiplier (RM) parameters of the model using the Kuenm package to obtain the parameter combination with the optimal goodness of fit for the input data. First, we constructed a large set of candidate models, then evaluated and selected the optimal model. All candidate models were generated by combining 17 regularization multiplier values (0.1 to 1 at 0.1 intervals, 2 to 6 at 1 intervals, plus 8 and 10) with all 29 possible feature class combinations (linear-L, quadratic-Q, hinge-H, product-P and threshold-T). Second, candidate models were screened by measuring statistical significance with the partial ROC (Receiver Operating Characteristic) value, assessing model prediction capability with the omission rate, and evaluating model complexity with the AICc (Akaike Information Criterion, corrected) value. The model parameter combination with the lowest AICc value (ΔAICc = 0) was selected as the optimal model [45]. After optimization, the parameters of MaxEnt model were set as RM = 0.2 and FC = LQP.
To improve prediction accuracy, 75% of the occurrence records were designated as training data, and the remaining portion was used as the final evaluation dataset for the model. The segmentation of training data and test data was repeated three times. For the configuration of pseudo-absence points, we select four candidate size gradients of 727 (consistent with the number of real existing points), 1000, 5000, and 10,000, and calculate the average True Skill Statistic (TSS) value across ten candidate models (see Table S4). The results show that when the number of pseudo-absence points is 5000, the average TSS of all models reaches the maximum, so this parameter is uniformly adopted for subsequent calculations [46,47]. The value of TSS ranges from −1 to 1. The closer this indicator is to 1, the better the simulation performance of the model [48,49]. The mean TSS value in this study is 0.882, indicating that our models achieve relatively high accuracy. For simulation studies, it is generally agreed that models with a TSS value greater than 0.8 exhibit excellent predictive performance; therefore, we only retain models with TSS scores greater than 0.8 for ensemble modeling [50,51]. In this study, we first used the Biomod2 package to simulate the suitable distribution of S. chinensis under current climate scenarios, and output continuous suitability raster layers (where each grid corresponds to a suitability probability value) and binary threshold layers (where 0 and 1 denote unsuitable and suitable areas, respectively). Next, we performed reclassification processing on the threshold layers in ArcMap 10.5, extracted the raster data of suitable habitats, and superimposed the continuous suitability raster layer using the extracted raster layer as a mask. Finally, we calculated the optimal threshold for distinguishing suitable areas from unsuitable areas, which is 0.471. Specifically, areas with a species occurrence probability equal to or greater than P (p ≥ P) are defined as suitable areas, while the remaining areas are classified as non-suitable areas. The study area was further divided into four categories: regions with p < 0.471 were classified as unsuitable areas; regions with 0.471 ≤ p < 0.55 were classified as low-suitability areas; regions with 0.55 ≤ p < 0.75 were classified as moderate-suitability areas; regions with 0.75 ≤ p < 0.986 were classified as high-suitability areas.
The above analysis only identifies climatically suitable areas for S. chinensis, and has not yet excluded areas unfavorable for the growth of S. chinensis such as water areas and cultivated land. Therefore, when formulating the planning for suitable habitats of S. chinensis, this study further integrates current and future land use data, and conducts spatial overlay between climatically suitable areas and natural forests (i.e., natural habitat types suitable for the growth of S. chinensis). The overlapping area obtained is defined as the suitable habitat of S. chinensis.

2.2. Correlation Analysis Between Environmental Variables and the Chemical Constituents of S. chinensis

To facilitate the application of research findings to practical production, it is necessary to identify which environmental factors may induce changes in the content of chemical constituents in medicinal plants. Accordingly, this study established a correlation analysis between environmental factors and active constituents.

2.2.1. Ranking of the Importance of Chemical Component Determination of S. chinensis in Heilongjiang Province and Related Environmental Factors

In this study, high-performance liquid chromatography was employed to determine 46 batches of wild S. chinensis samples collected across Heilongjiang Province, and the data were analyzed using the Similarity Evaluation System for Chromatographic Fingerprint of Traditional Chinese Medicine. For detailed methodological procedures, please refer to the Supporting Information of the chromatographic fingerprint. It is generally recognized that the determination of any single active component or index constituent cannot fully characterize the intrinsic quality of traditional Chinese medicine [52]. Principal Component Analysis (PCA) can extract several independent composite variables based on practical requirements, with the aim of retaining the maximum amount of information from the original variables. This method constitutes a scientifically valid dimensionality reduction technique [53]. Principal Component Analysis (PCA) was performed on the normalized peak areas of 9 common peaks from 46 samples using the R v4.1.2 software package. The eigenvalues, contribution rates and cumulative contribution rates were calculated, and the screening plot (Figure S1) was generated. To clarify the extent to which environmental variables influence the chemical constituents of S. chinensis, this study is based on the XGBoost-SHAP (eXtreme Gradient Boosting-SHapley Additive exPlanations analysis. Taking the response variable FD (peak area of each chemical component) as the stratification basis, the training set is extracted from the entire sample at a ratio of 70%, and model fitting is performed [54]. Model fitting adopts a pre-defined hyperparameter configuration, and the objective function is set as mean squared error. On the training set, by comparing the model prediction results with the measured values, the root mean squared error (RMSE), mean absolute error (MAE) and coefficient of determination (R2) are calculated to evaluate the in-sample fitting performance of the model. Furthermore, to analyze the influence mechanism of various environmental factors on FD, the SHAP value of each feature was calculated sample-by-sample by combining the TreeExplainer algorithm based on the trained model. Based on the mean absolute SHAP value corresponding to each feature, the global importance of environmental factors is obtained through sorting [55] (Table S5). To eliminate the interference from correlations among environmental variables on the subsequent calculation of the model, Pearson’s rank correlation analysis implemented in ENMTools v 1.0.4 was performed to retain environmental variables with high feature importance and low correlation coefficients (|r| < 0.8). The environmental factors retained for modeling in each component are shown in Table S6.

2.2.2. Construction of the Spatial Distribution Pattern of Chemical Constituents of S. chinensis in Heilongjiang Province

All-subsets regression analysis traverses all possible models and screens out the optimal model based on statistical criteria such as adjusted R2 and Mallows Cp. On this basis, the relative weight analysis method can be further applied to quantify the contribution degree of each variable to the explanatory power of the model [56]. Based on the sampling sites of S. chinensis in Heilongjiang Province and the calculation results of fingerprints, the environmental factor data corresponding to the coordinates of 46 samples and the peak area data of fingerprints were input into RStudio (2023.06.1+524). Using the MuMIn v 1.47.5 package, with corresponding environmental factors as independent variables (x), the comprehensive principal component (pc) with significant correlation with environmental variables and the peak areas of five chemical components (Schisandrol A, Gomisin A, Angeloylgomisin H, Schisantherin B, Schizandrin A and Schizandrin B) were taken as dependent variables (y) respectively, to construct the correlation between the chemical components of S. chinensis and environmental factors. The specific formula is as follows:
y = β1x1 + β2x2 + … + βixn
where y represents the content of chemical components, xn denotes environmental variables, and βi are regression coefficients, with results evaluated using the coefficient of determination (R2) and F-test [57]. Based on these results, the comprehensive principal component (pc) of S. chinensis’s comprehensive components and the spatial distribution of individual components were constructed using ArcGIS 10.5.

2.3. Planning of S. chinensis Protected Areas and Targeted Wild Tending in Heilongjiang Province

2.3.1. Protected Areas Planning

In protected area planning, to obtain climatically relatively stable suitable habitats for S. chinensis throughout the 21st century, we conducted spatial overlay of suitable distribution areas under 17 current and future climate scenarios, took the overlapping area as a template, uniformly masked the suitable habitat layers of all scenarios to the extent of this template, and finally imported the processed data into the Zonation 4.0 software platform to perform priority area ranking calculation. All layers are uniformly assigned a weight of 1, and the remaining parameters retain the model’s default settings. By setting the warp factor to “1” and adopting the cell-based removal strategy, the conservation planning results are further optimized [58]. Existing research shows that protecting 5–20% of habitats can enable the conservation of over 50% of species [59]. For practical considerations, the top 20% of ranked areas are delineated as protected reserves in accordance with the set objectives, and existing conservation gaps are identified synchronously. The output results are ultimately classified as follows: the top 5% is delineated as priority protection areas, 5% to 10% as general protection areas, and 10% to 20% as partial protection areas [60].

2.3.2. Targeted Wild Tending Planning

Wild tending of traditional Chinese medicinal materials is an ecological cultivation approach that closely mimics natural conditions. Rooted in the original habitat of the targeted species, this approach fully adheres to the biological laws of traditional Chinese medicinal materials on the premise of maintaining ecosystem stability. It primarily relies on natural ecological processes with minimal artificial intervention, thereby achieving the sustainable enhancement of the population productivity of geo-authentic crude drugs [6]. The core scientific objective of wild tending is to accurately quantify and elucidate the formation mechanism of the geo-authenticity of medicinal materials, thereby providing solid theoretical and data support for site selection decision-making of tending bases [61]. Meanwhile, Huang et al. proposed the concept of directional cultivation of Chinese medicinal materials, and highlighted that the selection of cultivation regions for Chinese medicinal materials is one of the most critical factors affecting the quality and yield of Chinese medicinal materials, and the selection of geo-authentic production regions is the most fundamental and critical principle for the cultivation of geo-authentic Chinese medicinal materials [62].
Based on the above analysis, the targeted wild tending area planned in this study aims to identify high-quality districts and counties for each chemical component of S. chinensis in Heilongjiang Province under various climate scenarios. Both the habitat suitability and medicinal quality of S. chinensis are taken into consideration for delineating this area. Accordingly, taking the suitable habitats of S. chinensis under each climate scenario as a mask, we conducted masking processing on the spatial distribution layers of each component content obtained in Section 2.2 respectively, and then input both datasets into Zonation for calculation. The parameter settings are completely consistent with those adopted in the priority protected area planning. Given that development and construction activities are prohibited within nature reserves, both the established nature reserves in Heilongjiang Province and the protected areas planned in this study are excluded from the output results of the Zonation software. The natural break method is based on the inherent natural grouping characteristics of data, realizes the optimal aggregation of homogeneous values by identifying classification intervals, and maximizes the differences between different categories [63]. Therefore, this study adopts the natural break method to divide the results into high-quality regions and general-quality regions. In China, local governments act as major participants in biodiversity conservation actions; accordingly, we conducted a county-scale hotspot analysis on the high-quality regions of wild S. chinensis populations in Heilongjiang Province, and finally obtained the hotspot districts and counties for targeted wild tending of each component of S. chinensis in Heilongjiang Province [64].

3. Results

3.1. Key Environmental Factors Driving S. chinensis Distribution and the Pattern of Its Potential Suitable Areas Under Current Climate Scenarios

Based on the calculation results from Biomod2, environmental factors with an average importance of >15% in model evaluation are defined as the primary environmental factors affecting the growth of S. chinensis. Ranked from highest to lowest importance, these factors are srad_winter, bio18, srad_summer, and bio13. The importance assessment of environmental factors used for modeling across each model is presented in Figure S2. By extracting 5000 random points from the current suitable habitat distribution for the four primary environmental variables, we obtained the following value ranges: srad_winter (Solar radiation from DEC to FEB) spans 4374–10,109 kJ·m−2·day−1, bio18 (Precipitation of warmest quarter) spans 218.819–1032.41 mm, srad_summer (Solar radiation from JUN to AUG) spans 14,746–19,921 kJ·m−2·day−1, and bio13 (Precipitation of wettest month) spans 118.458–611.194 mm (Table S7).
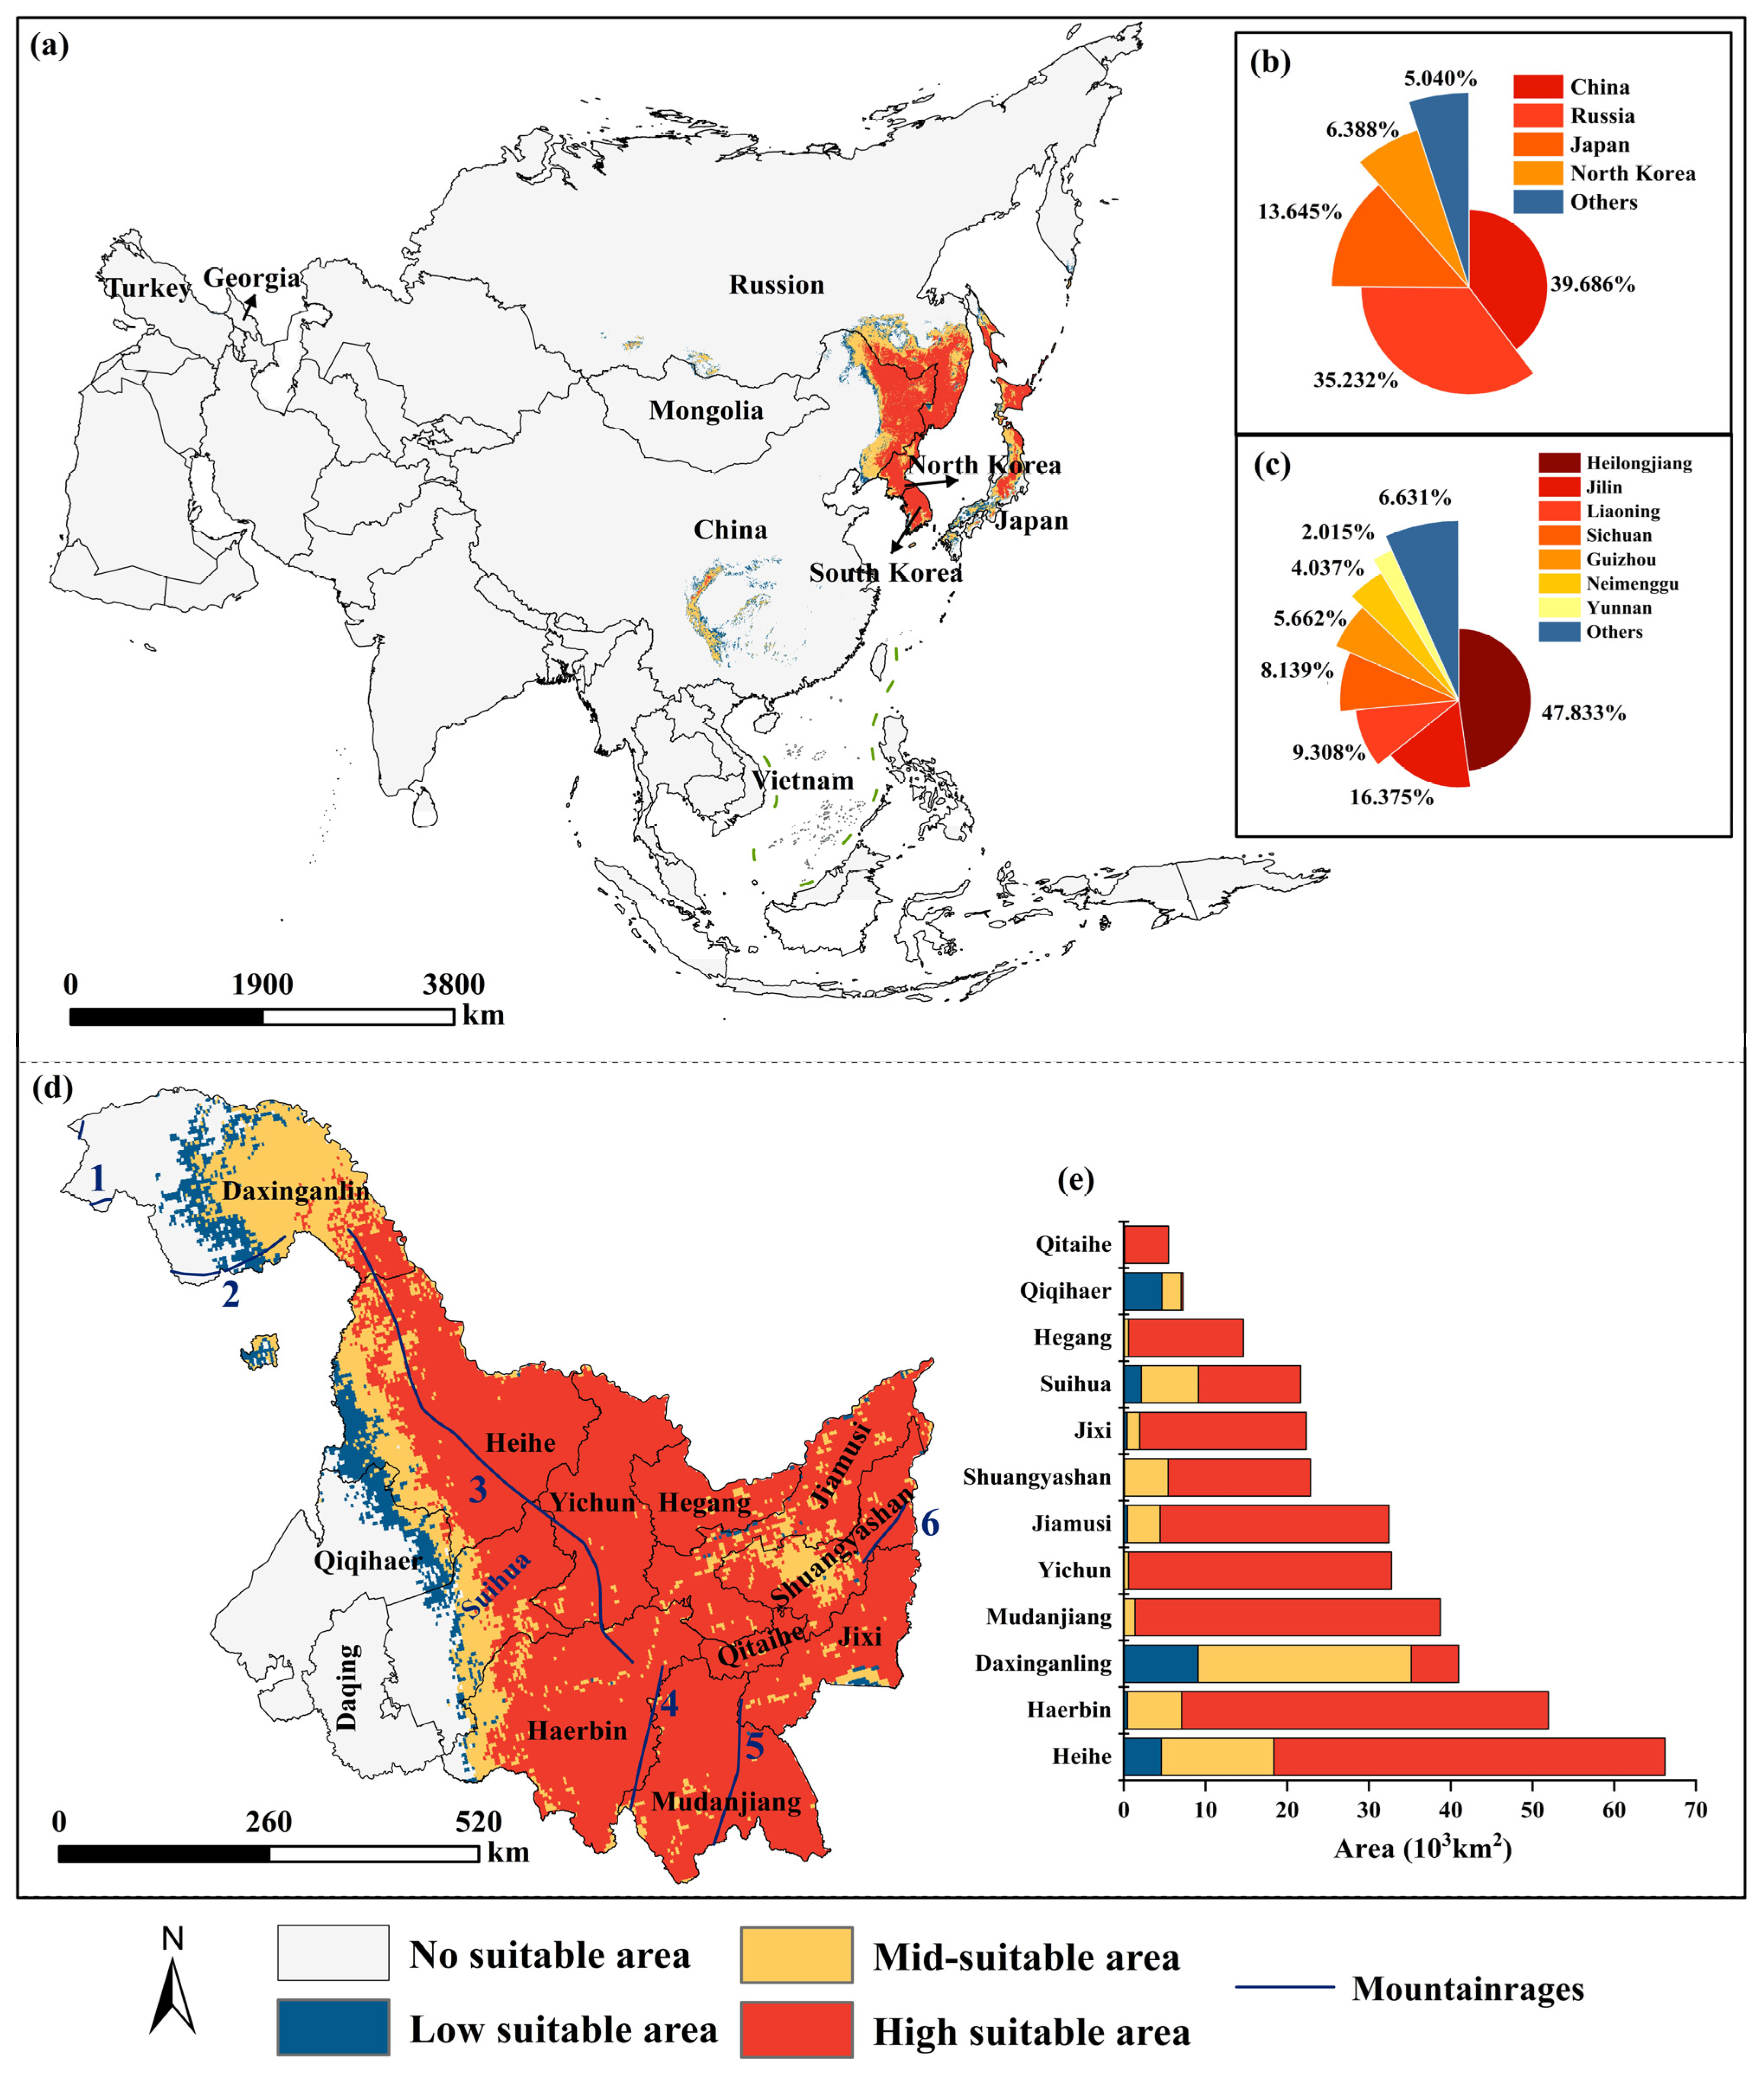
As shown in Figure 2, the simulation results obtained via Biomod2 indicate that the total suitable area of S. chinensis is 18.780 × 10⁵ km2. Among the three suitability grades, the highly suitable habitat has the largest area at 9.947 × 10⁵ km2, accounting for 52.964% of the total suitable habitat area; it is followed by the moderately suitable habitat, with an area of 6.233 × 10⁵ km2, accounting for 33.188% of the total suitable habitat area; the lowly suitable habitat has the smallest area of 2.601 × 10⁵ km2, accounting for 13.848% of the total suitable habitat area, as shown in Figure S3a. Within the entire ecological niche (Asia) of S. chinensis, the suitable habitat area in China is the largest at 7.453 × 10⁵ km2, accounting for 39.686% of the total suitable habitat area, as shown in Figure S3b.
Within the territory of China, the suitable distribution areas of S. chinensis are concentrated in Northeast China, including Heilongjiang Province, Jilin Province, Liaoning Province and eastern Inner Mongolia. Among these regions, Heilongjiang Province has the largest total suitable area for S. chinensis, which is 3.562 × 10⁵ km2, accounting for 47.833% of the total suitable area in China, as shown in Figure 2c. The area of highly suitable habitats for S. chinensis in Heilongjiang Province is 2.660 × 10⁵ km2, the area of moderately suitable habitats is 0.687 × 10⁵ km2, and the area of lowly suitable habitats is 0.215 × 10⁵ km2. The suitable distribution range of S. chinensis in Heilongjiang Province is relatively broad. Except for the western grasslands and the northernmost regions, all other areas are suitable for its distribution, and the highly suitable habitats are concentrated in mountainous areas, as shown in Figure 2d,e.

3.2. Key Environmental Factors Driving the Distribution of S. chinensis and Patterns of Its Potential Suitable Areas in Heilongjiang Province Under Future Climate Scenarios

Under future climate scenarios, among the four key environmental factors driving the distribution of S. chinensis, bio13 and bio18 will vary with carbon emission scenarios and the passage of time. Compared with current conditions, the average value of bio13 (precipitation of the wettest month) decreases across all future climate scenarios. Among different carbon emission scenarios, all but the SSP1-2.6 climate scenario show an increasing trend over time; the SSP1-2.6 scenario exhibits a trend of increasing first, followed by decreasing, then increasing again. Compared with current conditions, the average value of bio18 (precipitation of the warmest quarter) increases across all future climate scenarios. Among different carbon emission scenarios, all but the SSP1-2.6 climate scenario show a continuous increasing trend over time, while the SSP1-2.6 scenario presents a trend of increasing first and decreasing afterward (Figure S4).
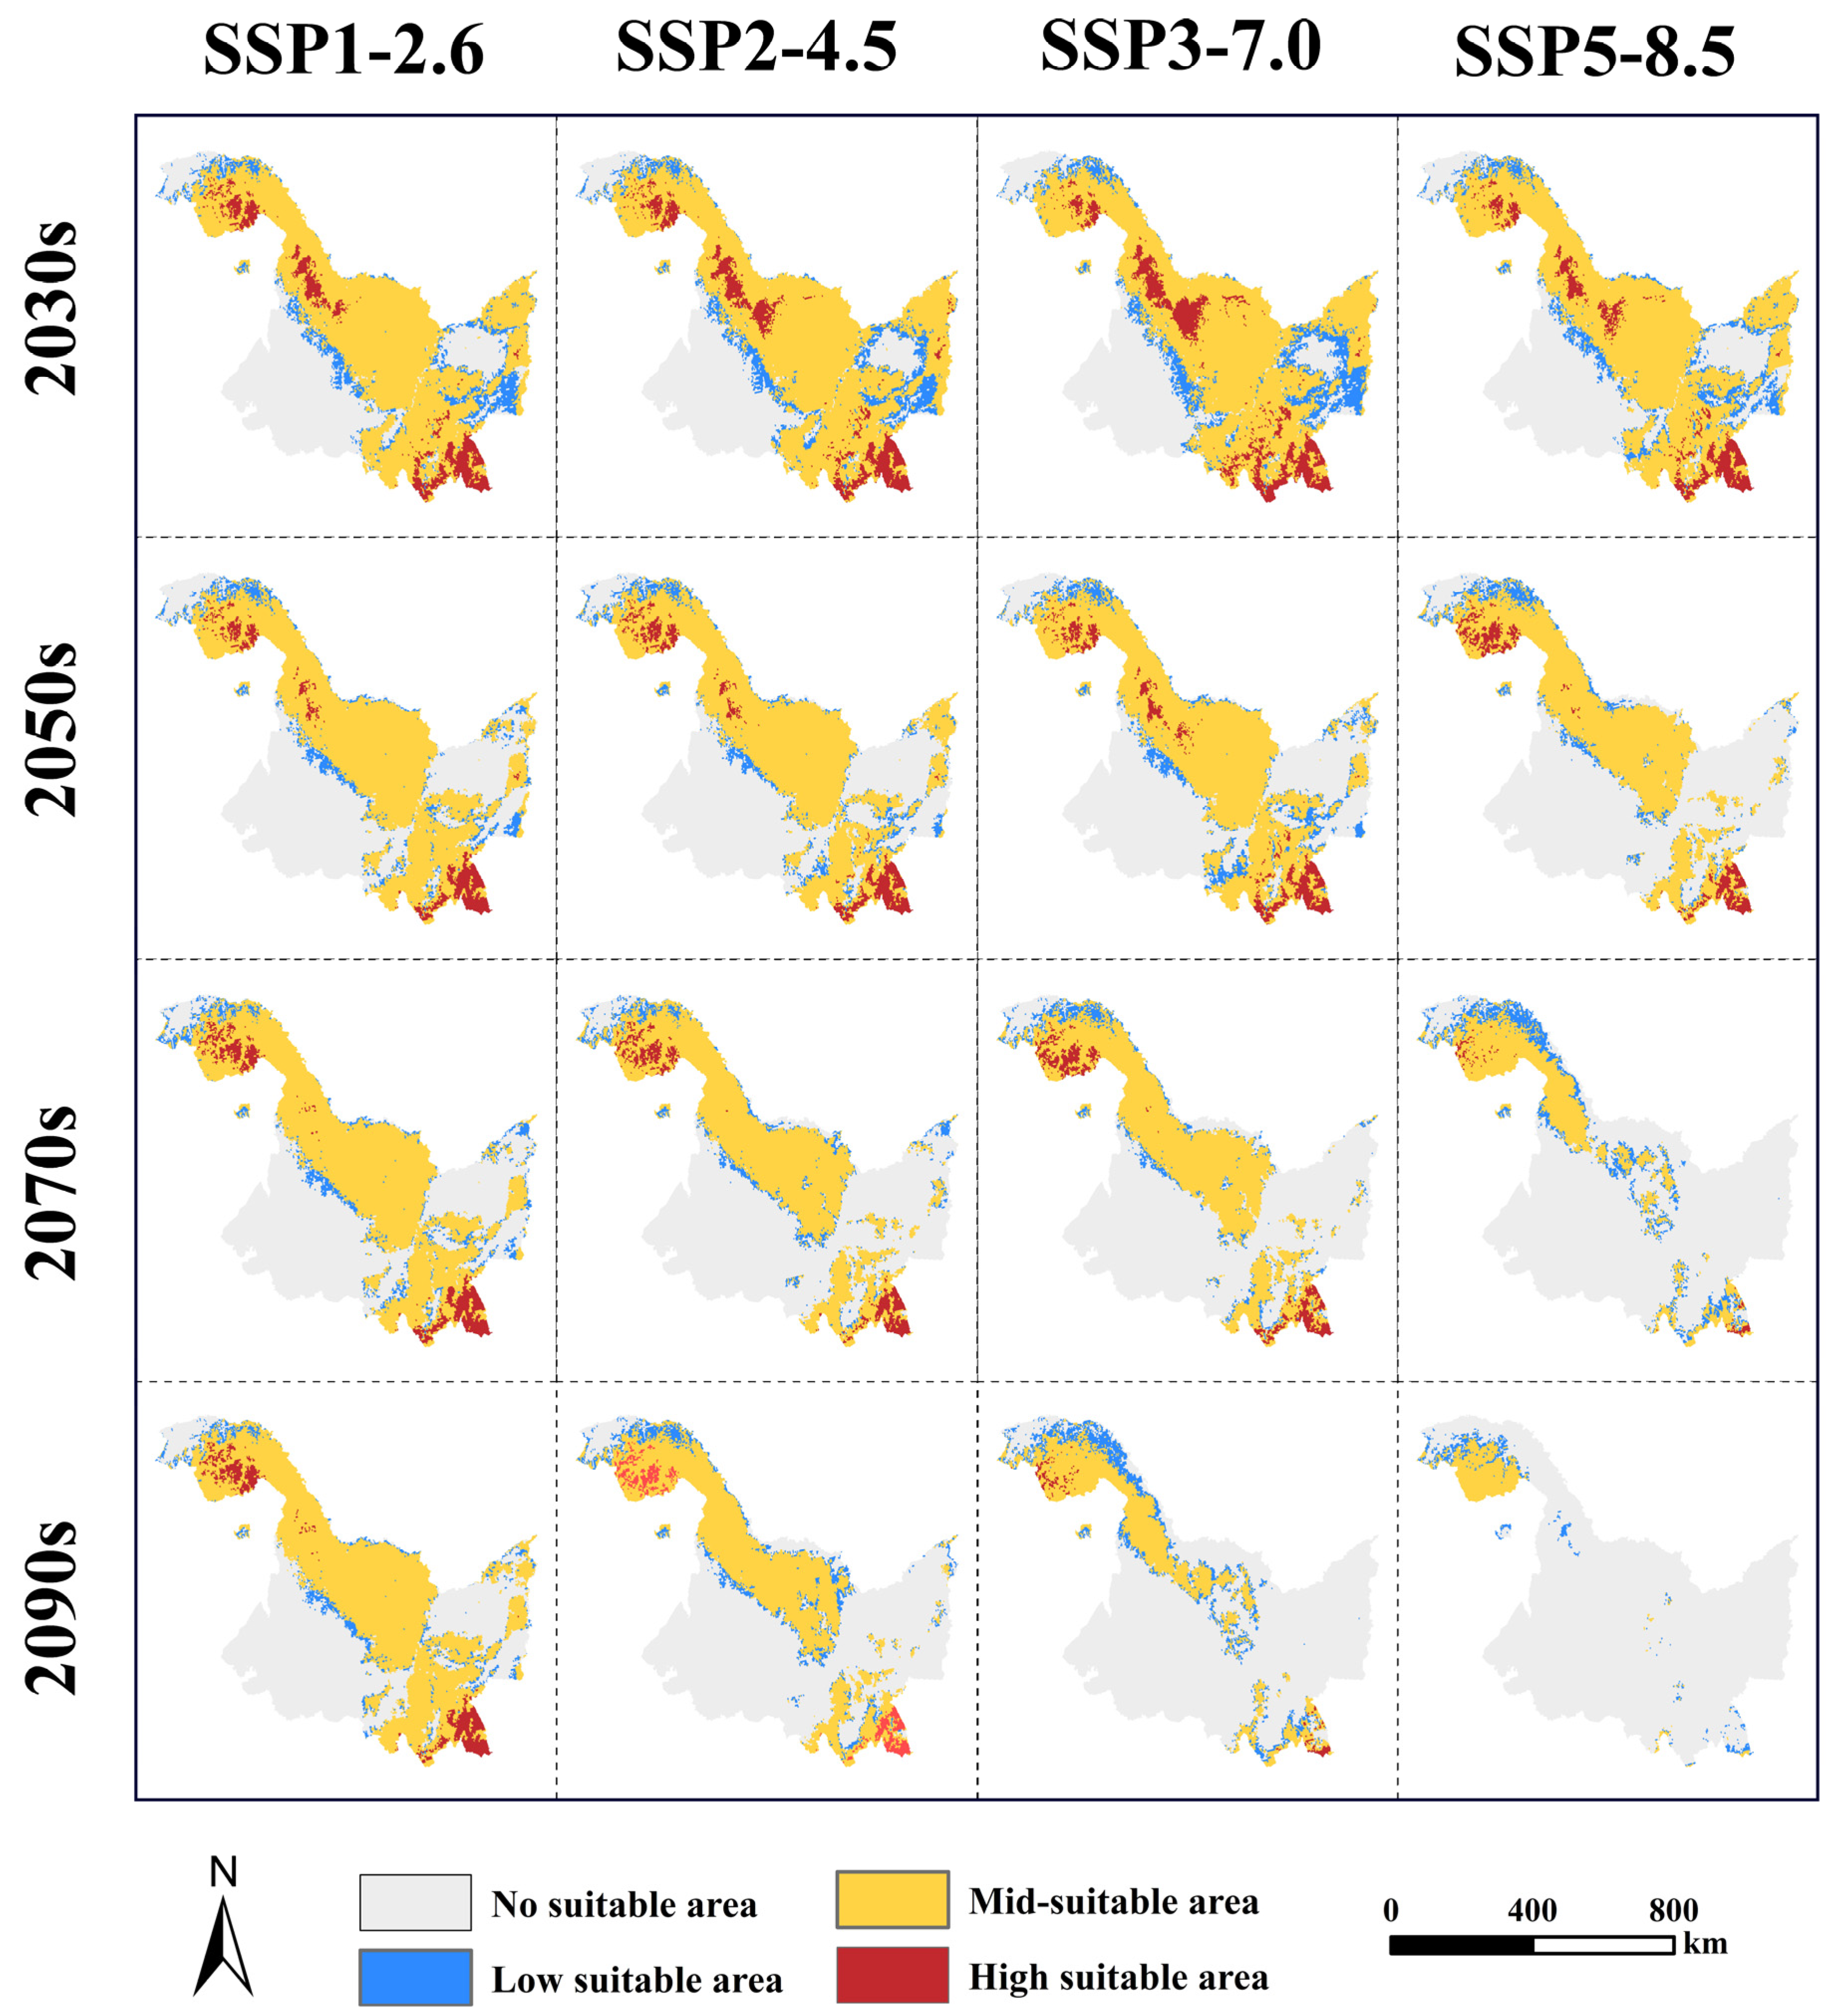
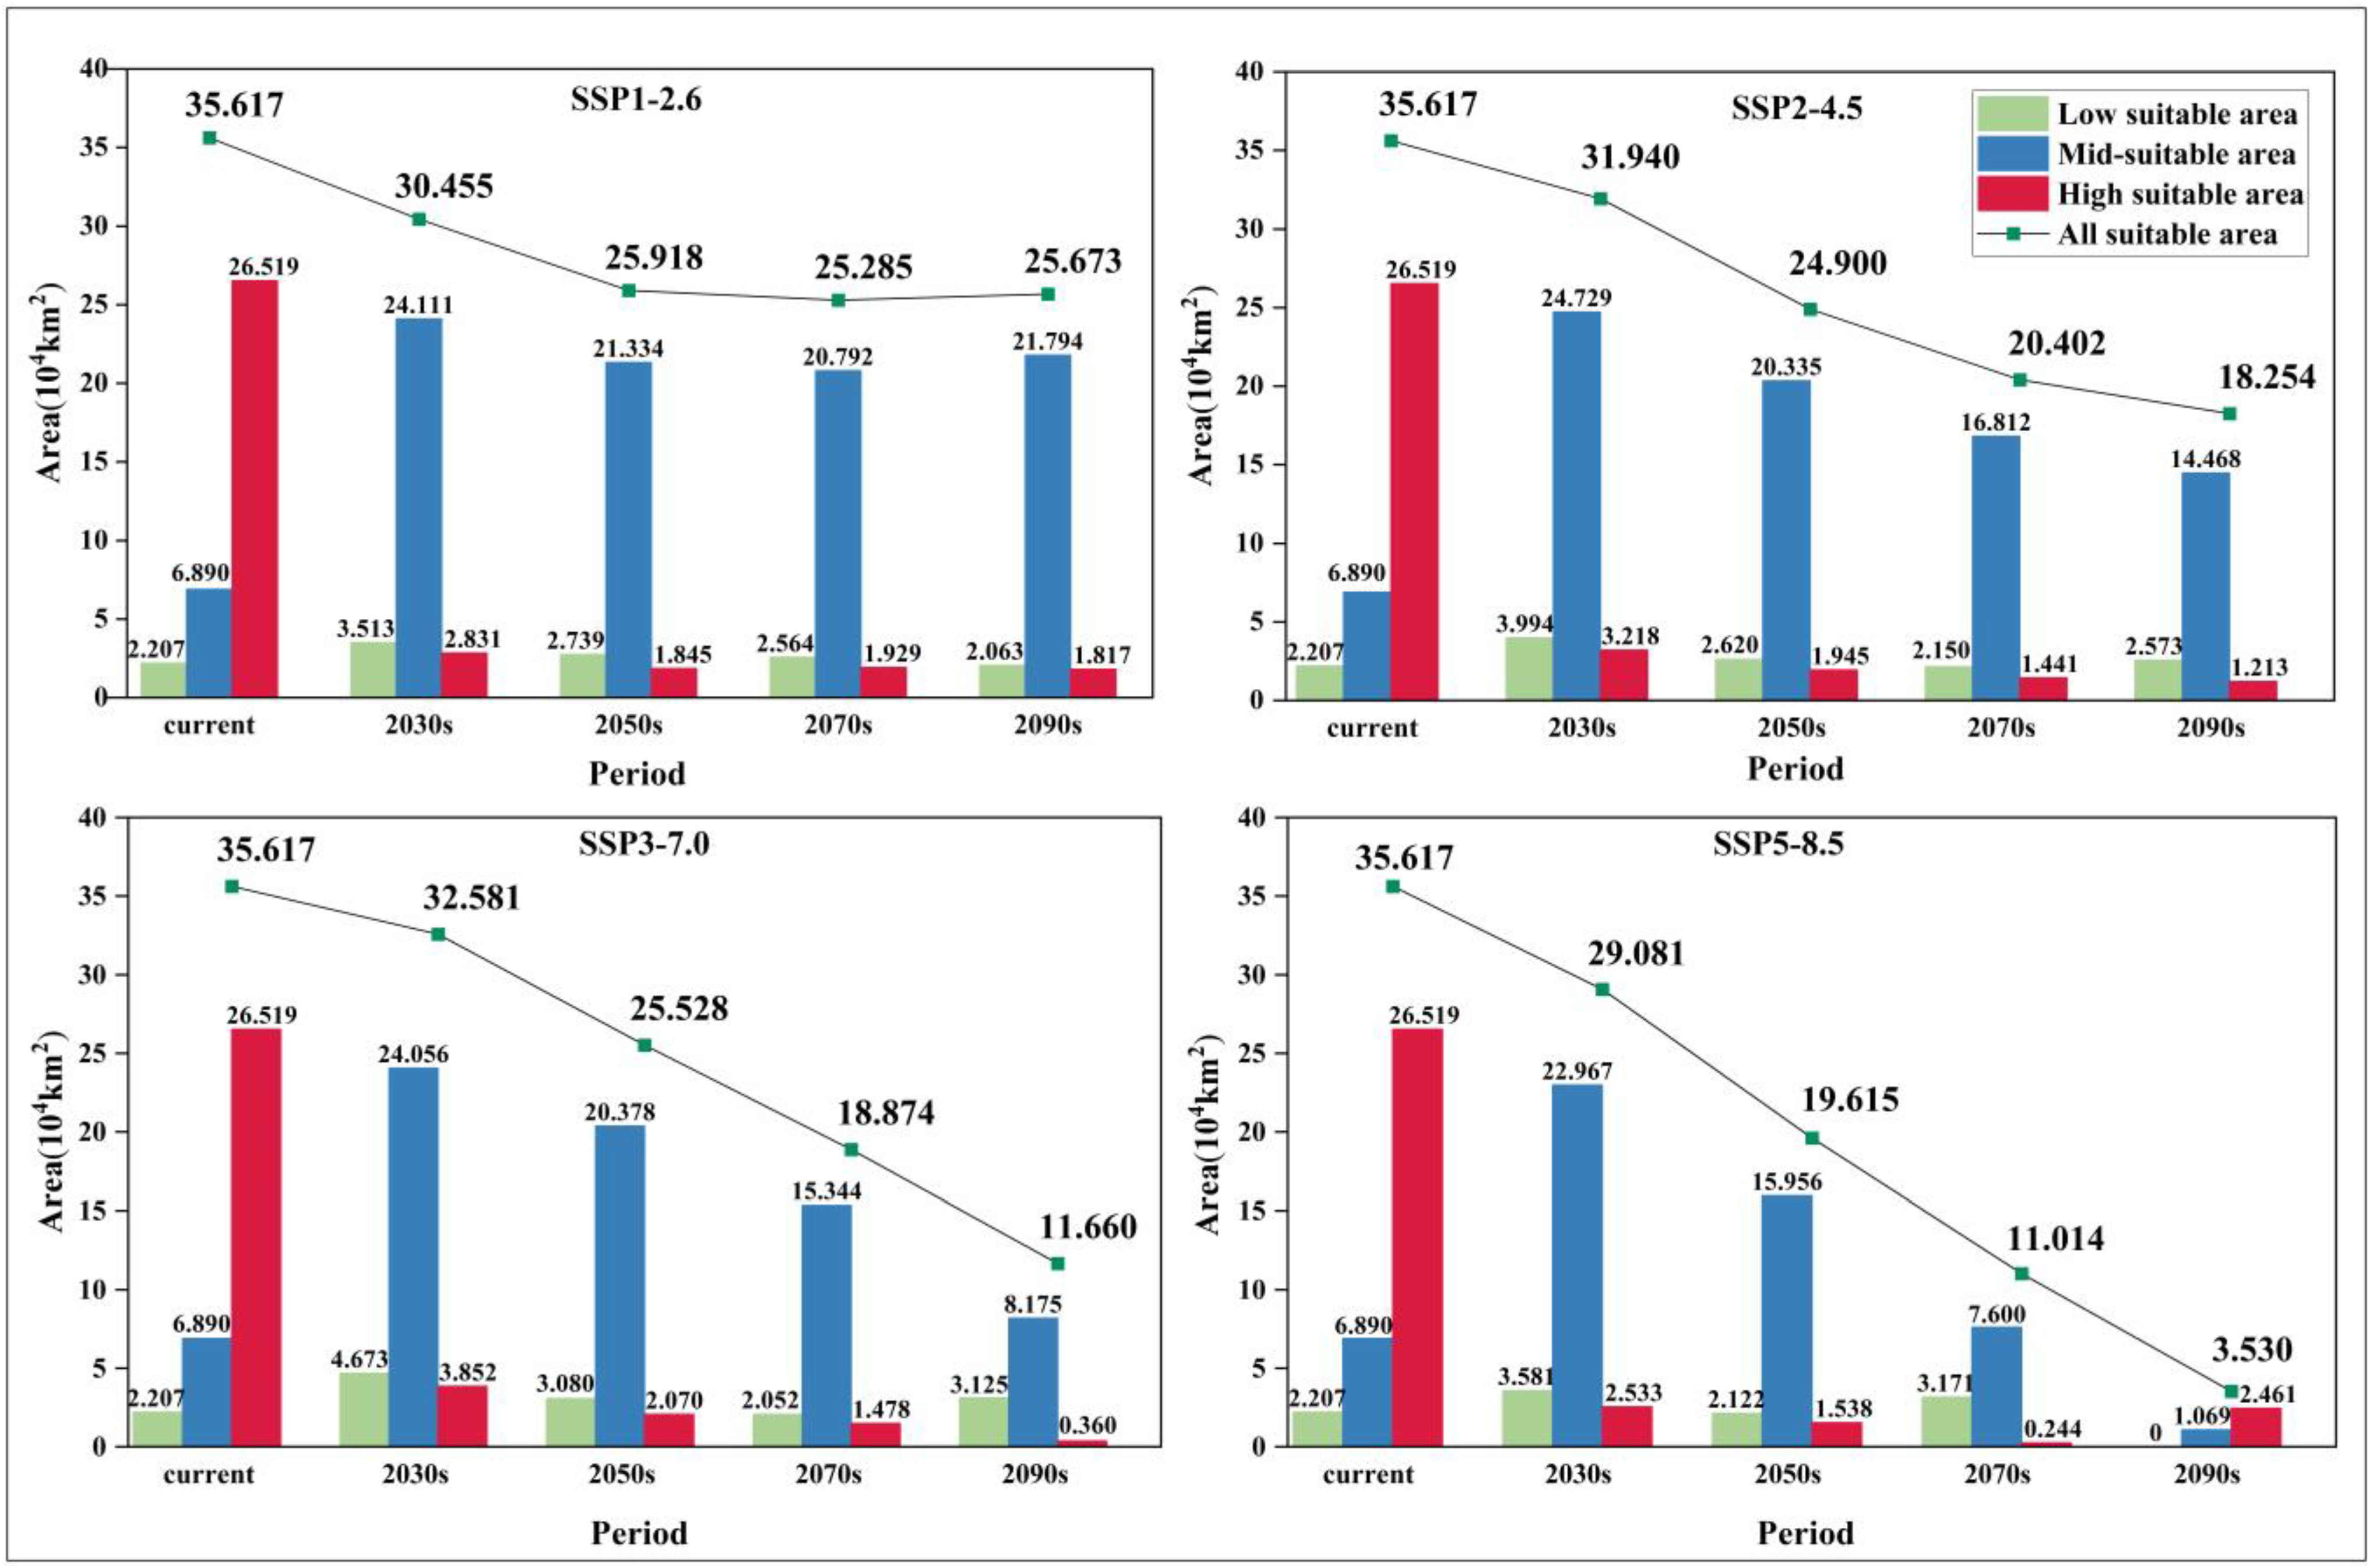
Under future climate change scenarios, the total area of suitable areas for S. chinensis in Heilongjiang Province will decrease year by year toward the northwest with the increase in years and carbon emissions (Figure 3). It is projected that under the SSP5-8.5 climate scenario for the 2090s, the area of suitable habitats for S. chinensis will shrink to the minimum, approximately 3.530 × 10⁴ km2, accounting for only 9.912% of the current area of suitable areas. Moreover, the low-suitability areas for S. chinensis will disappear completely under this scenario. Except that the current suitable areas are dominated by high-suitability areas, the pattern of suitable areas under various future climate scenarios will shift to being dominated by medium-suitability areas (Figure 4).

3.3. Dynamic Prediction of the Area of Suitable Habitats for S. chinensis in Heilongjiang Province Under Different Climate Scenarios

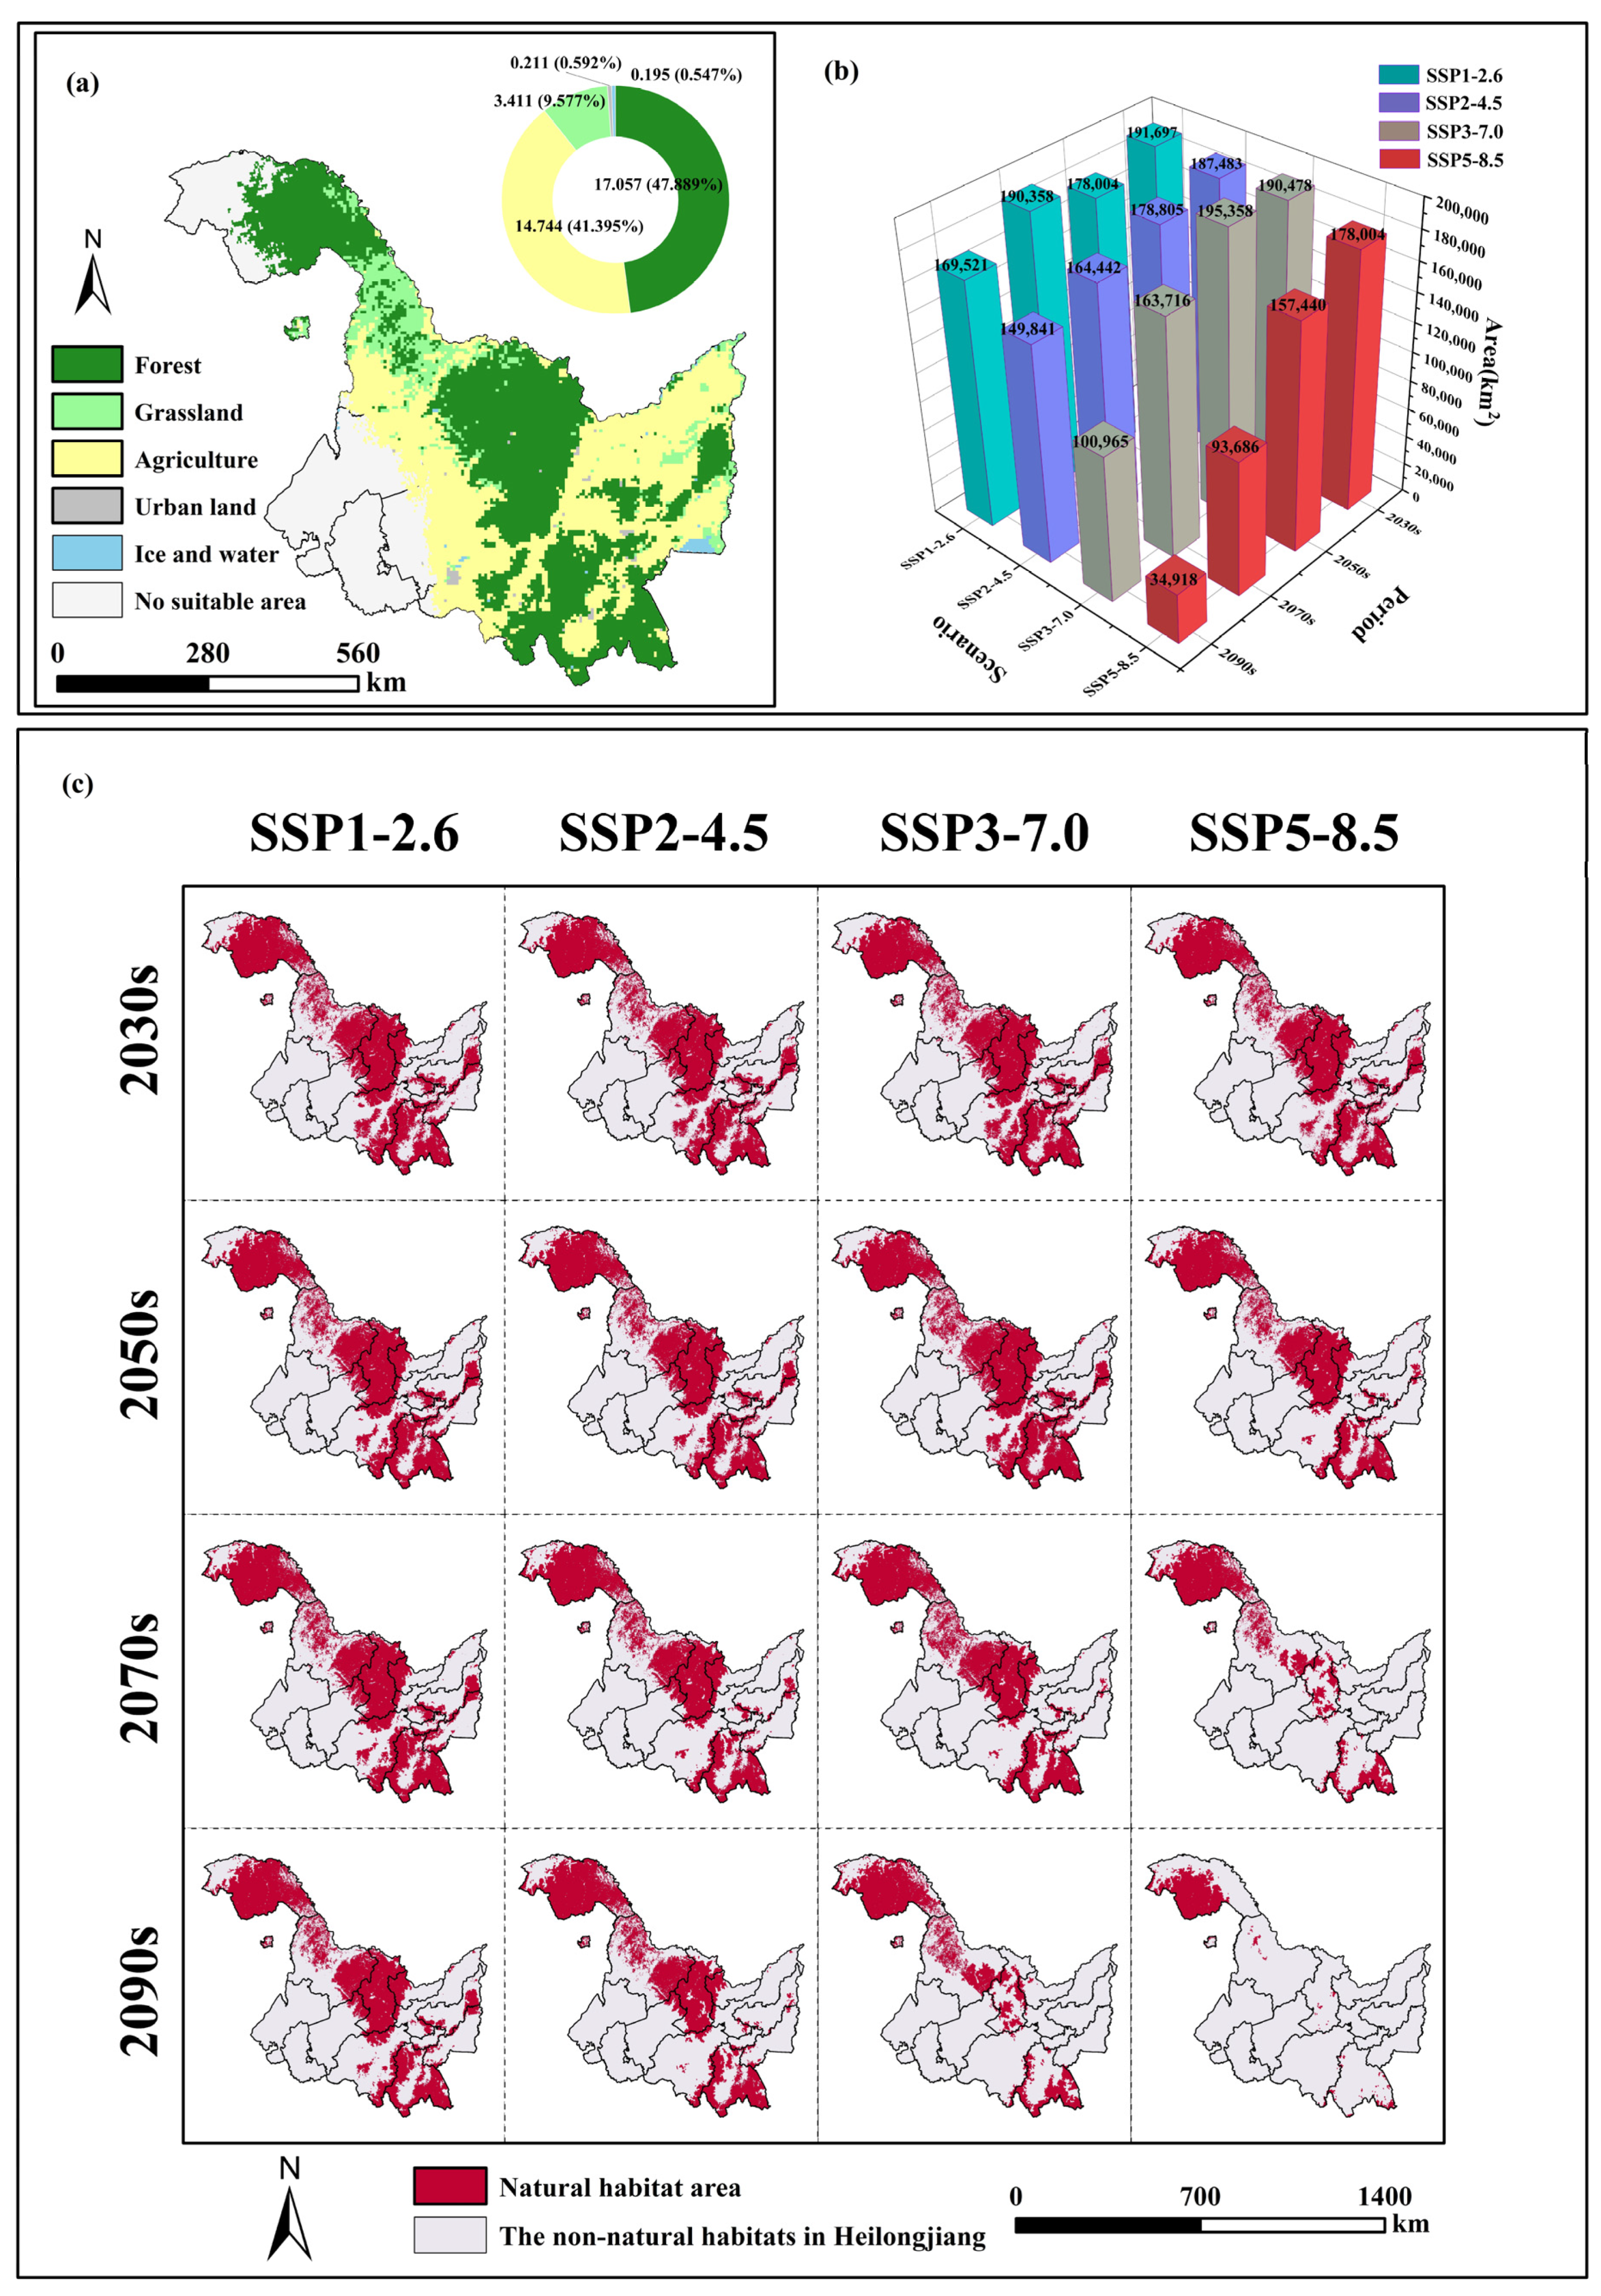
Forest land constitutes the primary habitat for S. chinensis under natural conditions. Under the current climate scenario, the forest land area within the suitable distribution range of S. chinensis in Heilongjiang Province is approximately 1.706 × 10⁵ km2, accounting for 47.891% of the total suitable distribution area (Figure 5a). In this study, the woodland located within the suitable distribution range is defined as the suitable habitat of S. chinensis. Based on the distribution of suitable distribution range of S. chinensis and the changes in woodland area in Heilongjiang Province under future climate scenarios, the future suitable habitat of S. chinensis in Heilongjiang Province can be obtained. Under the SSP1-2.6 and SSP2-4.5 carbon emission scenarios, the area of suitable habitats for S. chinensis in Heilongjiang Province will remain basically stable from the 2030s to the 2090s compared with that under the current climate scenario. However, under the SSP3-7.0 carbon emission scenario, the area of suitable habitats for S. chinensis in Heilongjiang Province shows a significant trend of increasing first and then decreasing. Under the SSP5-8.5 carbon emission scenario, the area of suitable habitats presents a gradual decreasing trend with the increase in years. It is projected that under the SSP5-8.5 climate scenario in the 2090s, only 3.492 × 10⁴ km2 of suitable habitats for S. chinensis will remain within Heilongjiang Province, accounting for only 20.471% of the current area of suitable habitats for S. chinensis in Heilongjiang Province (Figure 5b,c) (Table S8).

3.4. Establishment of HPLC Fingerprint of S. chinensis Medicinal Material, Identification of Characteristic Peaks and Similarity Evaluation of 46 Batches of Samples

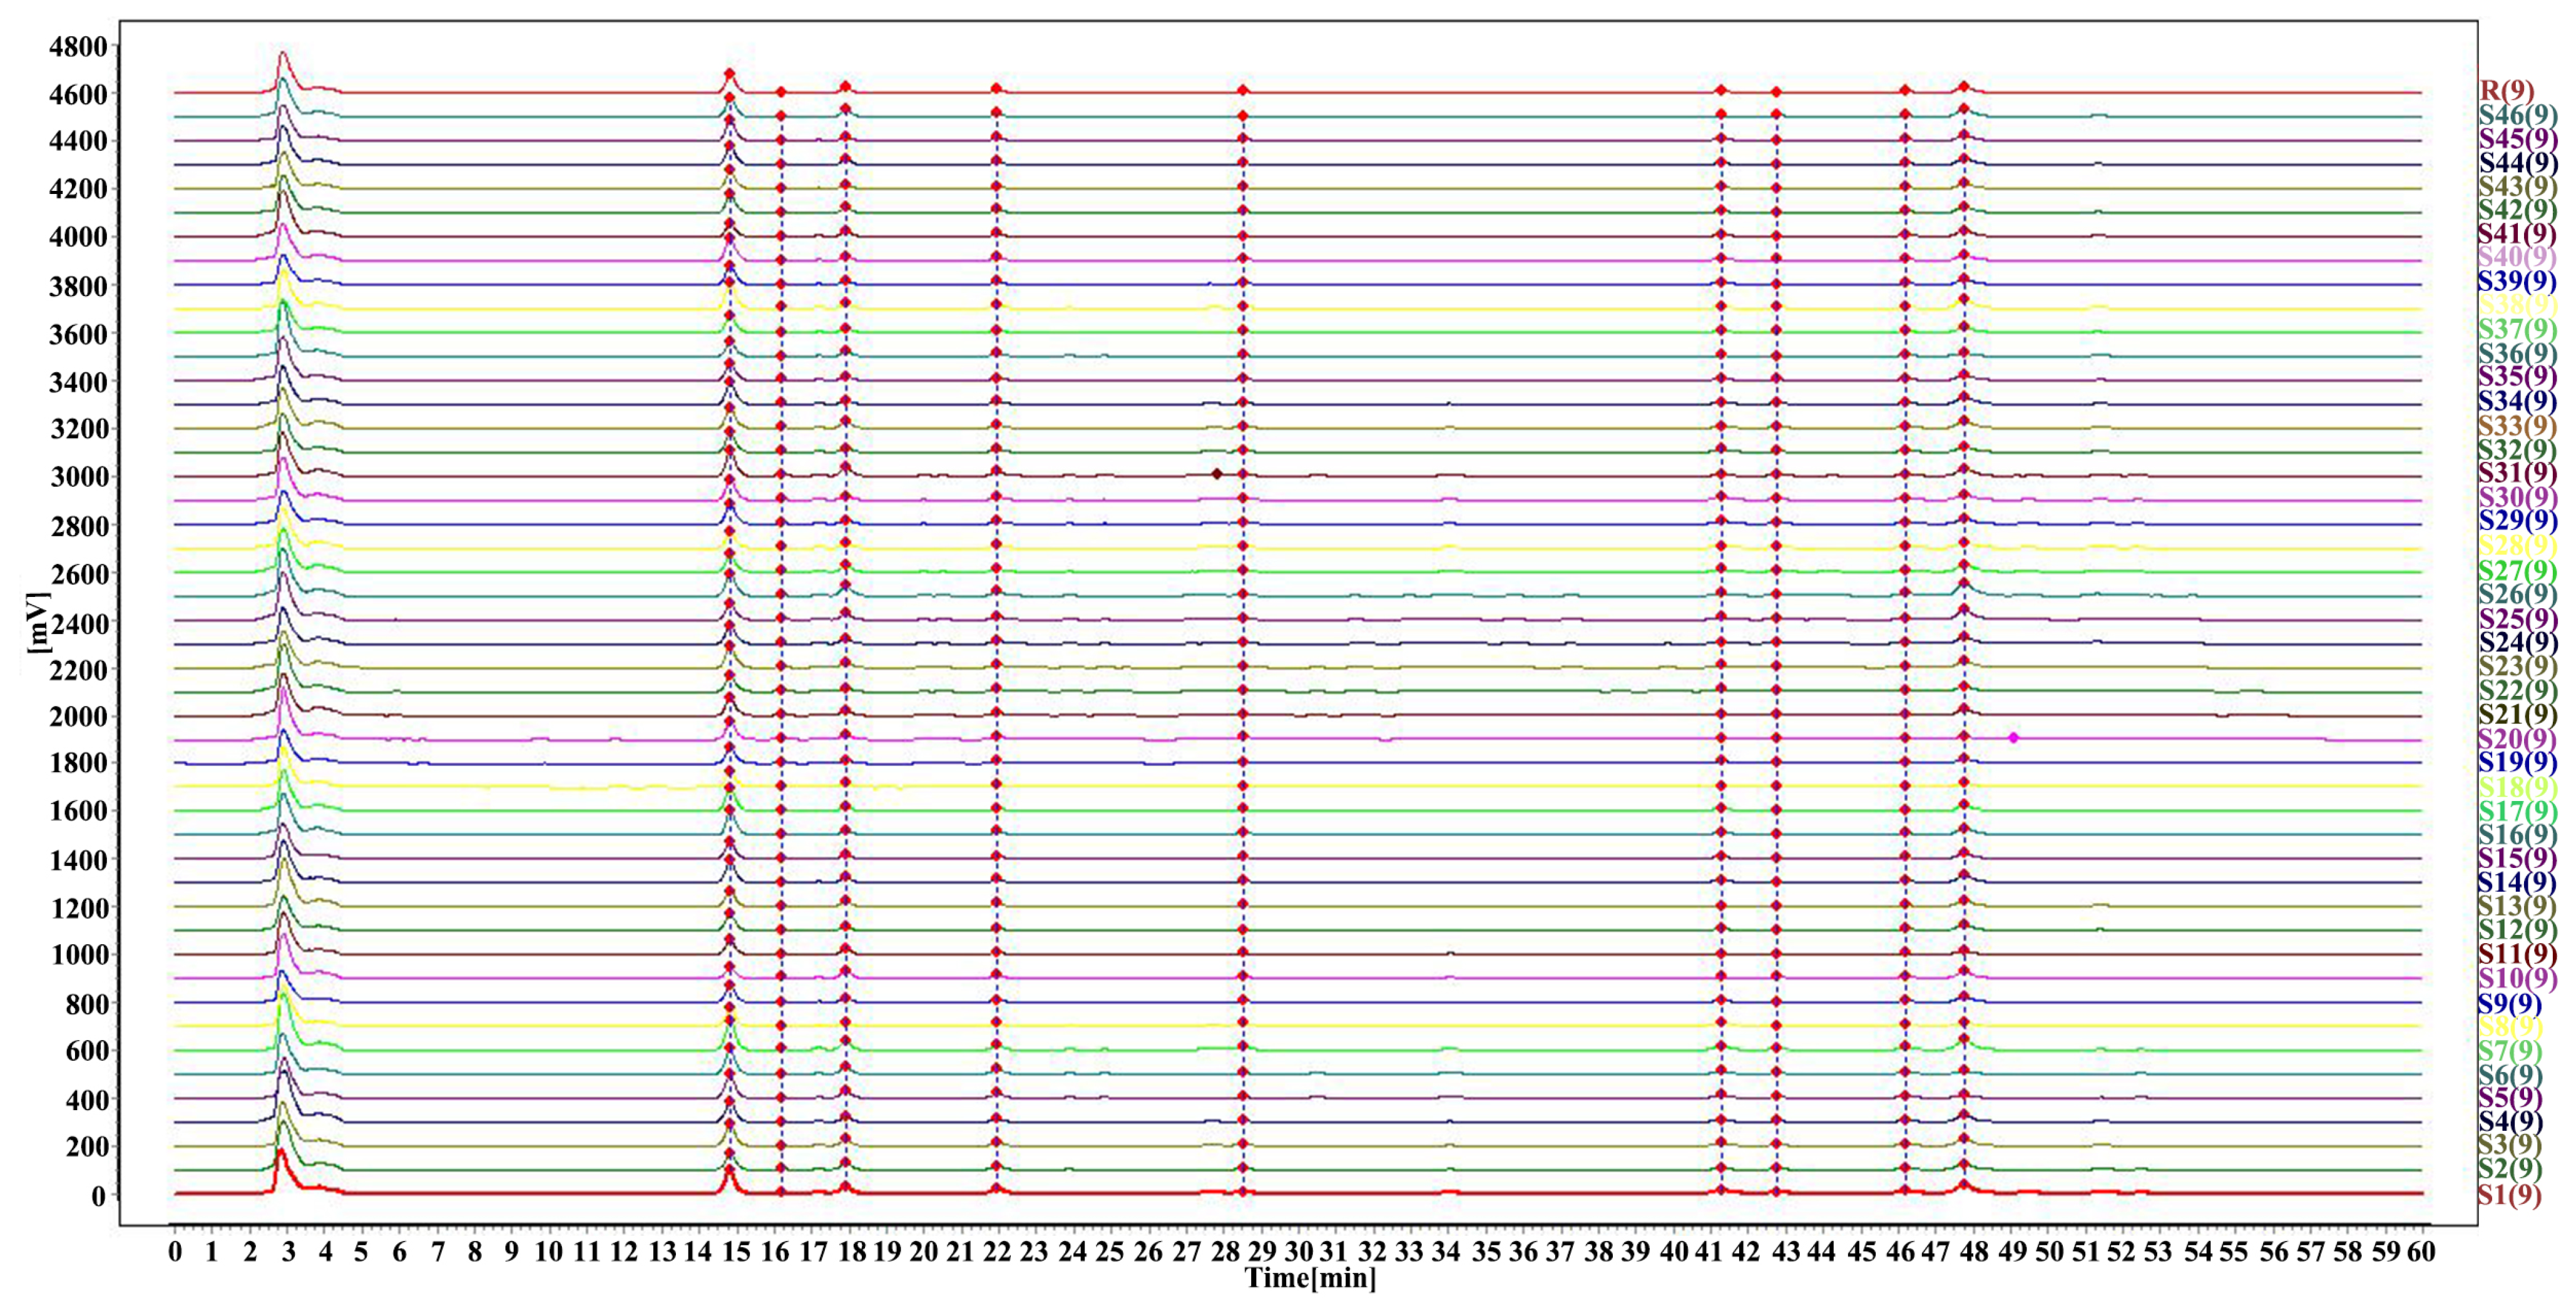
The Similarity Evaluation System for Chromatographic Fingerprint of Traditional Chinese Medicine (Version 2012) was adopted. Taking the chromatogram of the reference substance as the reference, the control reference fingerprint was generated by fitting the chromatograms of 15 batches of test samples (see Supporting Information of The Chromatographic Fingerprint). The fitting result is shown in Supporting Information of The Chromatographic Fingerprint. After fitting, a total of 18 common peaks were obtained. According to the chromatographic profiles of each sample, in addition to six components (Schisandrol A, Gomisin A, Angeloylgomisin H, Schizandrin B, Schisantherin B, Schizandrin A) whose chromatographic peaks have been located with reference standards, another three chromatographic peaks with good resolution, large peak area and stable retention were selected as characteristic peaks, and identification was performed by calculating the relative retention time of each characteristic peak with respect to the peak of Schisandrol A. A total of nine characteristic peaks are presented in Supporting Information of The Chromatographic Fingerprint. The baseline of the chromatogram is stable, with a large number of peaks, favorable response performance, good peak symmetry, and high resolution. Based on the optimal experimental conditions obtained in the Supporting Information of the fingerprint, the fingerprint construction was performed for 46 batches of S. chinensis, and the result is shown in Figure 6. The similarity evaluation results are presented in Figure S5. The similarity between the 46 batches of S. chinensis samples and the reference chromatogram ranged from 0.838 to 1. The similarity values for S. chinensis from Tangyuan County, Bayan County, and Wuchang City were only 0.838 and 0.840, indicating relatively low similarity, whereas those from Youhao District, Jinlin District, Suifenhe City, Hailin City, Sunwu County, Bei’an City, and Aihui District reached 1, showing extremely high similarity. These results indicate that the quality of S. chinensis medicinal materials varies among different regions.

3.5. Spatial Prediction Analysis of Chemical Constituents in S. chinensis from Heilongjiang Province

After XGBoost-SHAP analysis, the importance ranking of 34 environmental factors meeting the criteria was obtained. After removing environmental factors with a correlation ≥ 0.80 between any two factors and that had lower importance, the significant environmental factors associated with the comprehensive principal component (pc) of S. chinensis constituents and each individual constituent were identified (Table S6).
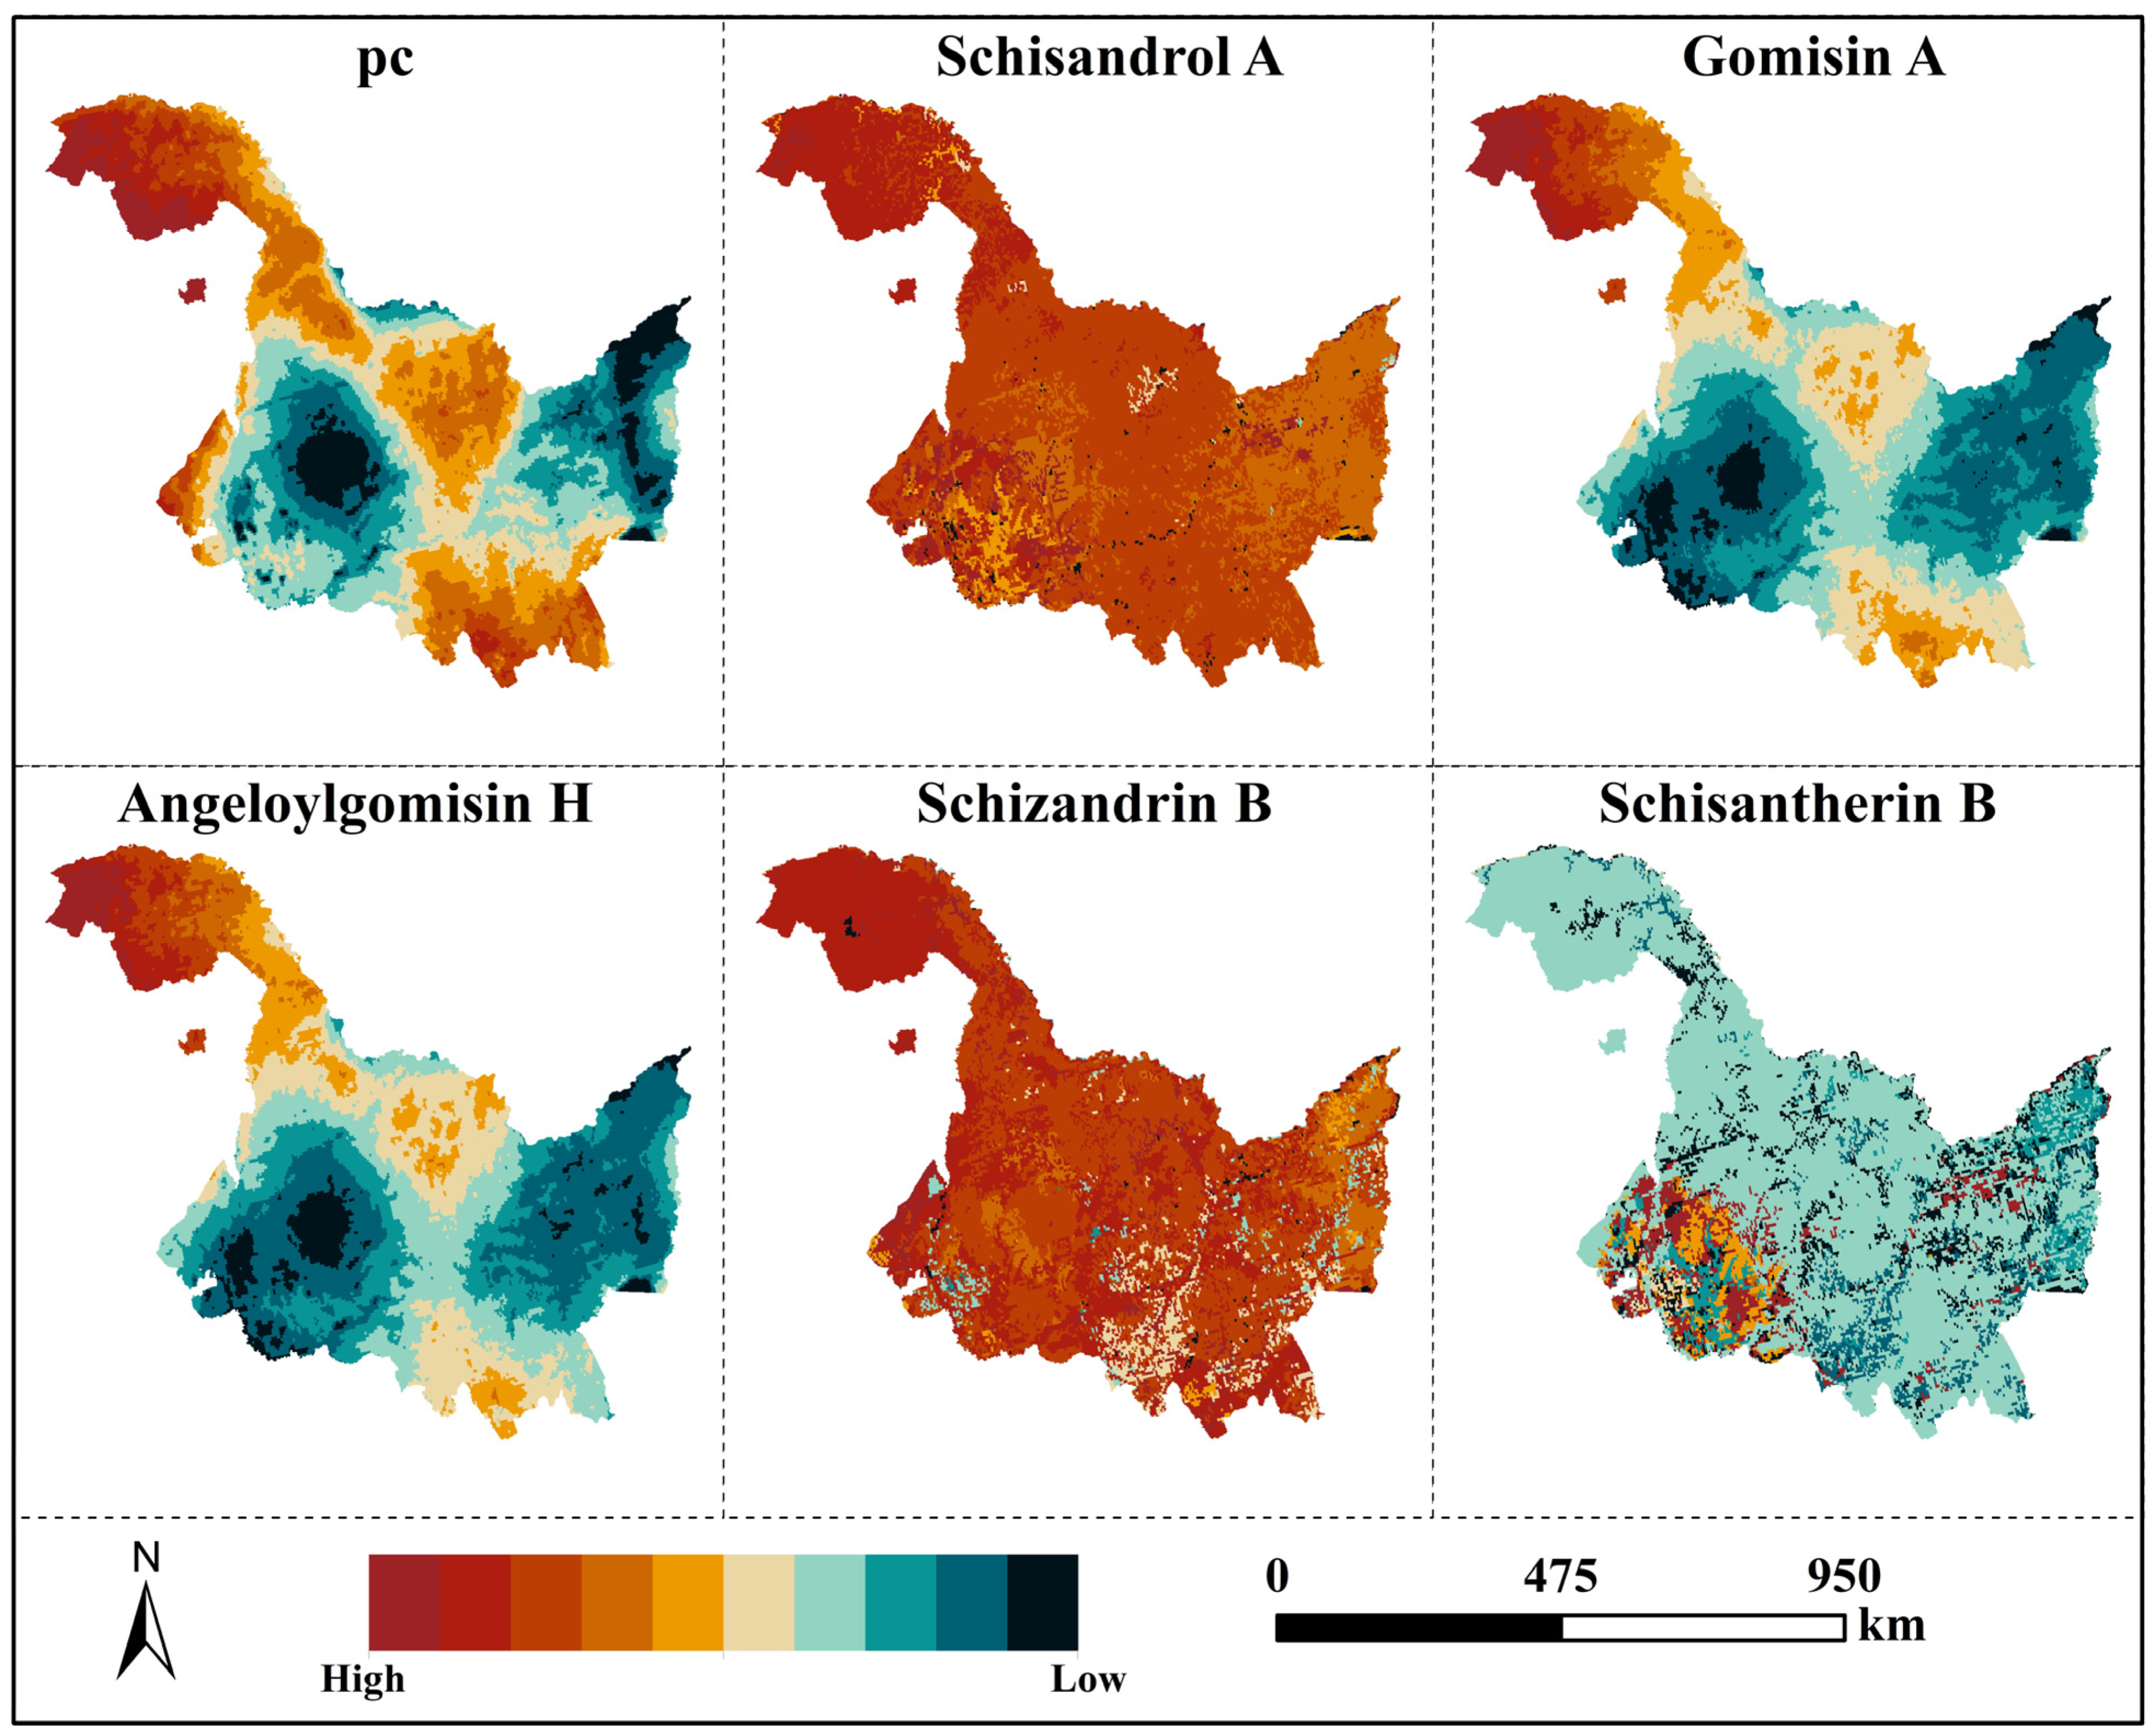
Within Heilongjiang Province, China, the MuMIn package was employed to construct the optimal mathematical correlation model between the fingerprint analysis results and environmental factors. To elucidate the correlation between the spatial distribution of medicinal component contents and environmental factors, the correlation model selects the optimal regression model based on the F-test p-value and adjusted R2; its formula, adjusted R2, and p-value are given in Table 2. The derived formula was employed to construct the spatial distribution patterns of the comprehensive components and individual components of S. chinensis in Heilongjiang Province. Based on the obtained spatial distribution patterns, the current high-quality distribution of the comprehensive components of S. chinensis is concentrated in the Greater Khingan Range and Lesser Khingan Range, and exhibits a patchy distribution in the Zhangguangcai Range and Laoye Range; the current high-quality distribution areas of Schisandrol A in Heilongjiang Province are widely distributed across various regions of the province; the high-quality distribution areas of Gomisin A are mainly concentrated in the Greater Khingan Range, with sporadic distribution in partial areas of the Lesser Khingan Range, Zhangguangcai Range and Laoye Range; the high-quality distribution areas of Angeloylgomisin H are mainly concentrated in the Greater Khingan Range, with sporadic distribution in partial areas of the Lesser Khingan Range, Zhangguangcai Range and Laoye Range; the high-quality distribution areas of Schizandrin B are widely distributed across various regions of Heilongjiang Province; the high-quality distribution areas of Schisantherin B are concentrated in southwestern Heilongjiang, presenting a patchy distribution (Figure 7).
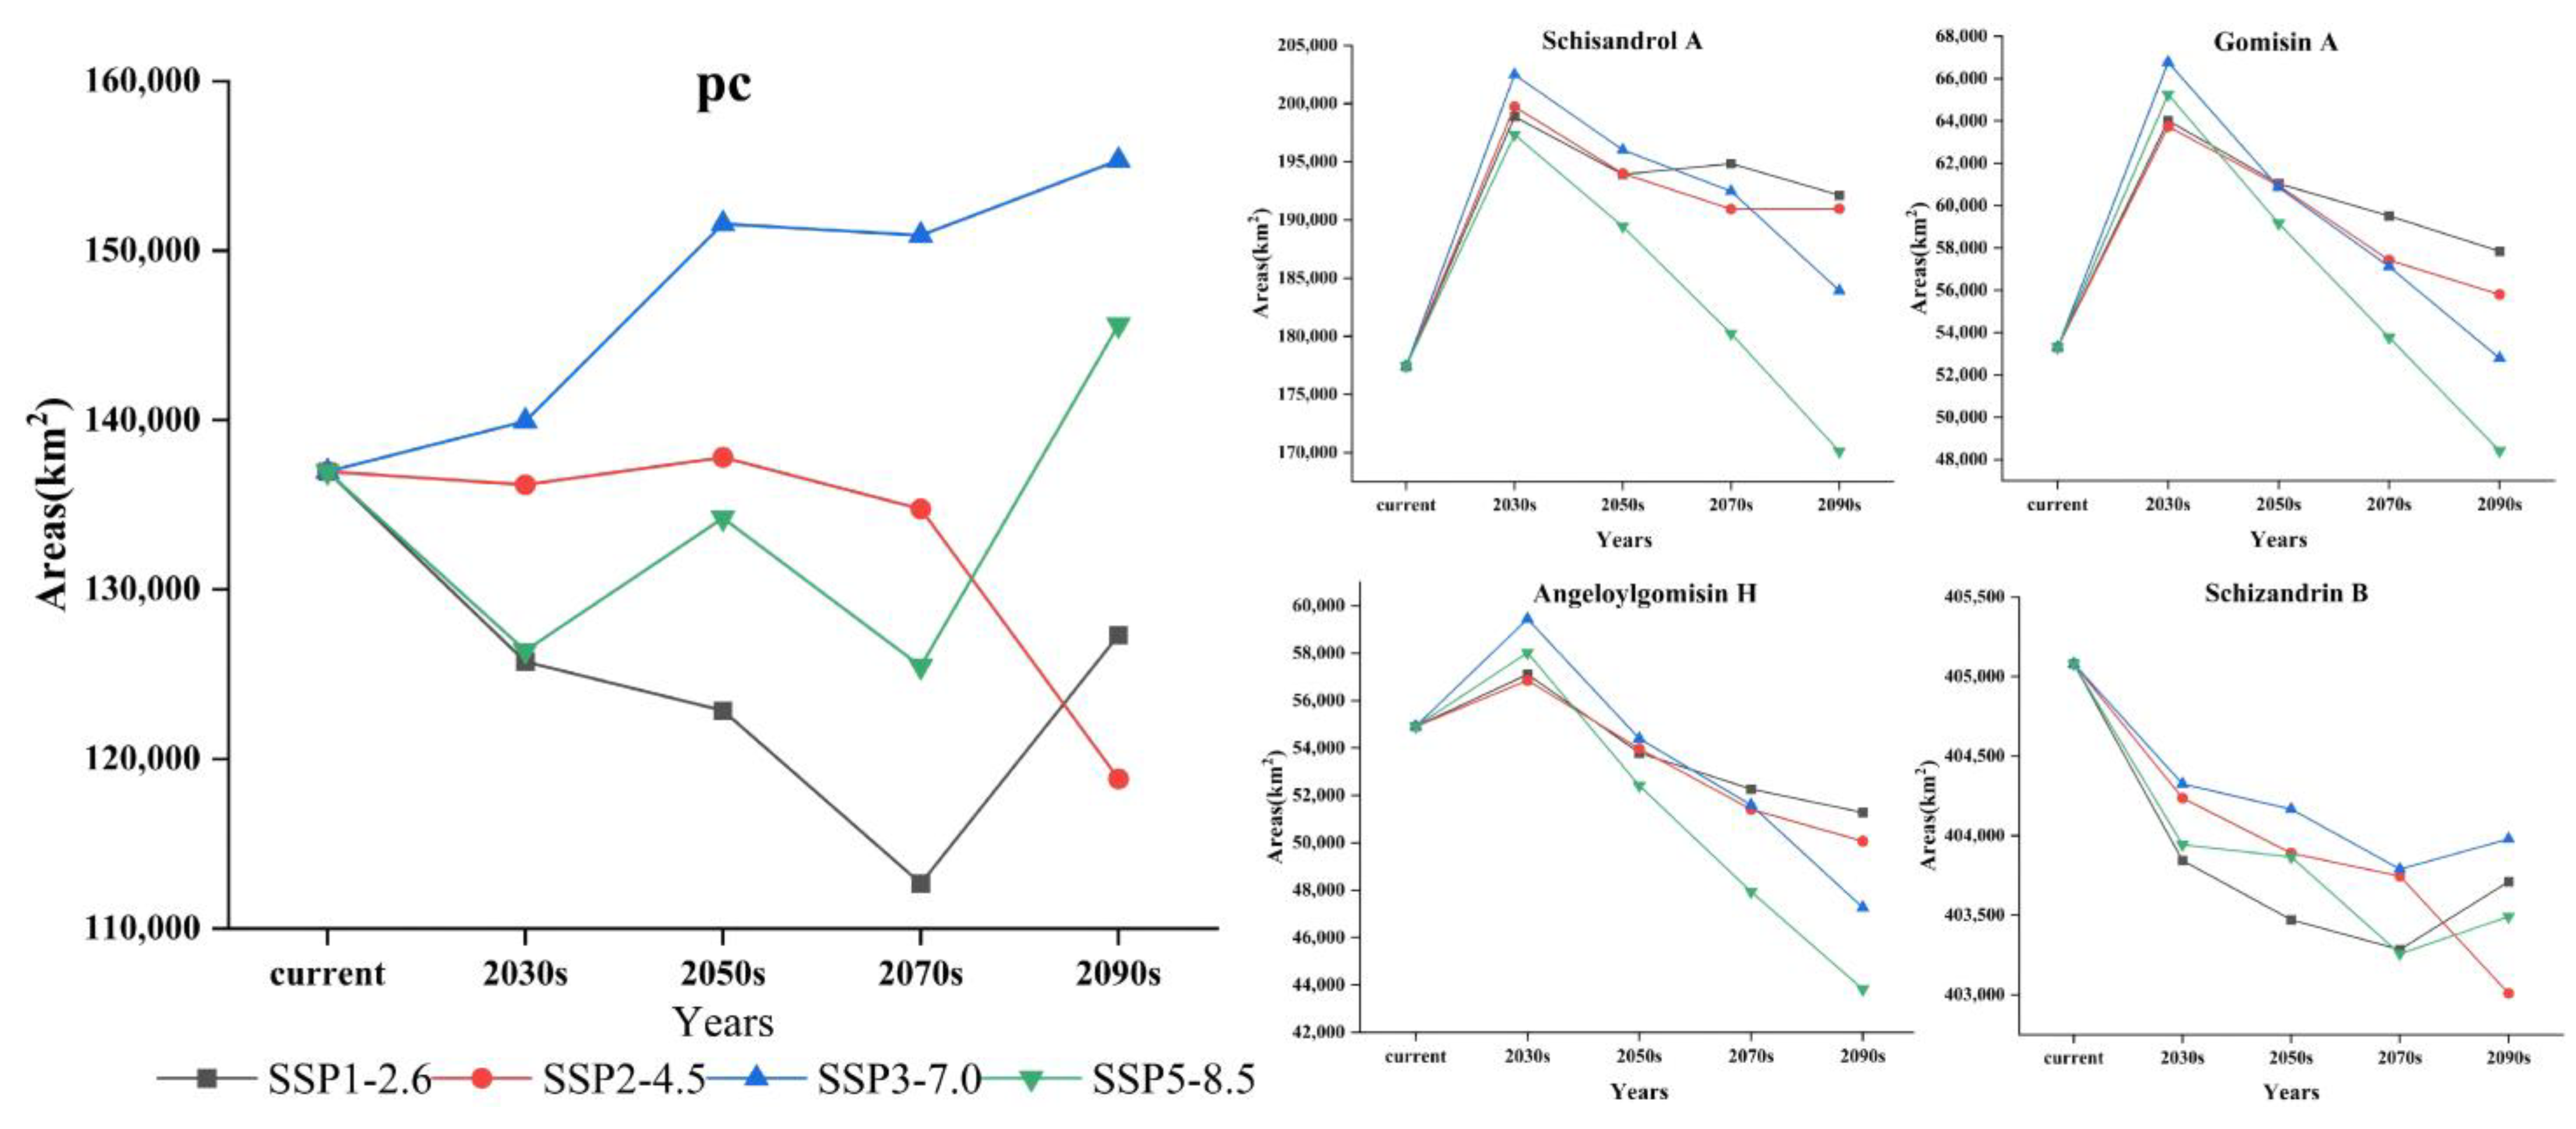
Under future climate change scenarios, the changes in the areas of high-quality regions for the comprehensive components and individual components of S. chinensis in Heilongjiang Province are shown in Figure 8. It can be observed that the future change trends in the areas of high-quality regions for the comprehensive components and individual components of S. chinensis in Heilongjiang Province differ from one another. Except for the climate scenario SSP3-7.0, the area of high-quality distribution regions of the comprehensive quality of S. chinensis shows an overall shrinking trend compared with the current climate scenario across all other scenarios; the area of high-quality distribution regions of Schisandrol A and Gomisin A shows an overall expanding trend compared with the current climate scenario under future climate scenarios; except for the 2030s period, the area of high-quality distribution regions of Angeloylgomisin H shows an overall shrinking trend compared with the current climate scenario under future climate scenarios; the area of high-quality distribution regions of Schizandrin B shows an overall shrinking trend compared with the current climate scenario under future climate scenarios. In addition, the content of Schisantherin B is only significantly correlated with the soil factor t_ph_H2O, and this soil factor is not projected to undergo substantial changes in the future [65]. Therefore, it can be concluded that the high-quality distribution area of Schisantherin B in S. chinensis in Heilongjiang Province will remain stable.

3.6. Planning for S. chinensis Protected Areas and Targeted Wild Tending Areas in Heilongjiang Province Under Global Change

3.6.1. Planning for S. chinensis Protected Areas in Heilongjiang Province Under Global Change

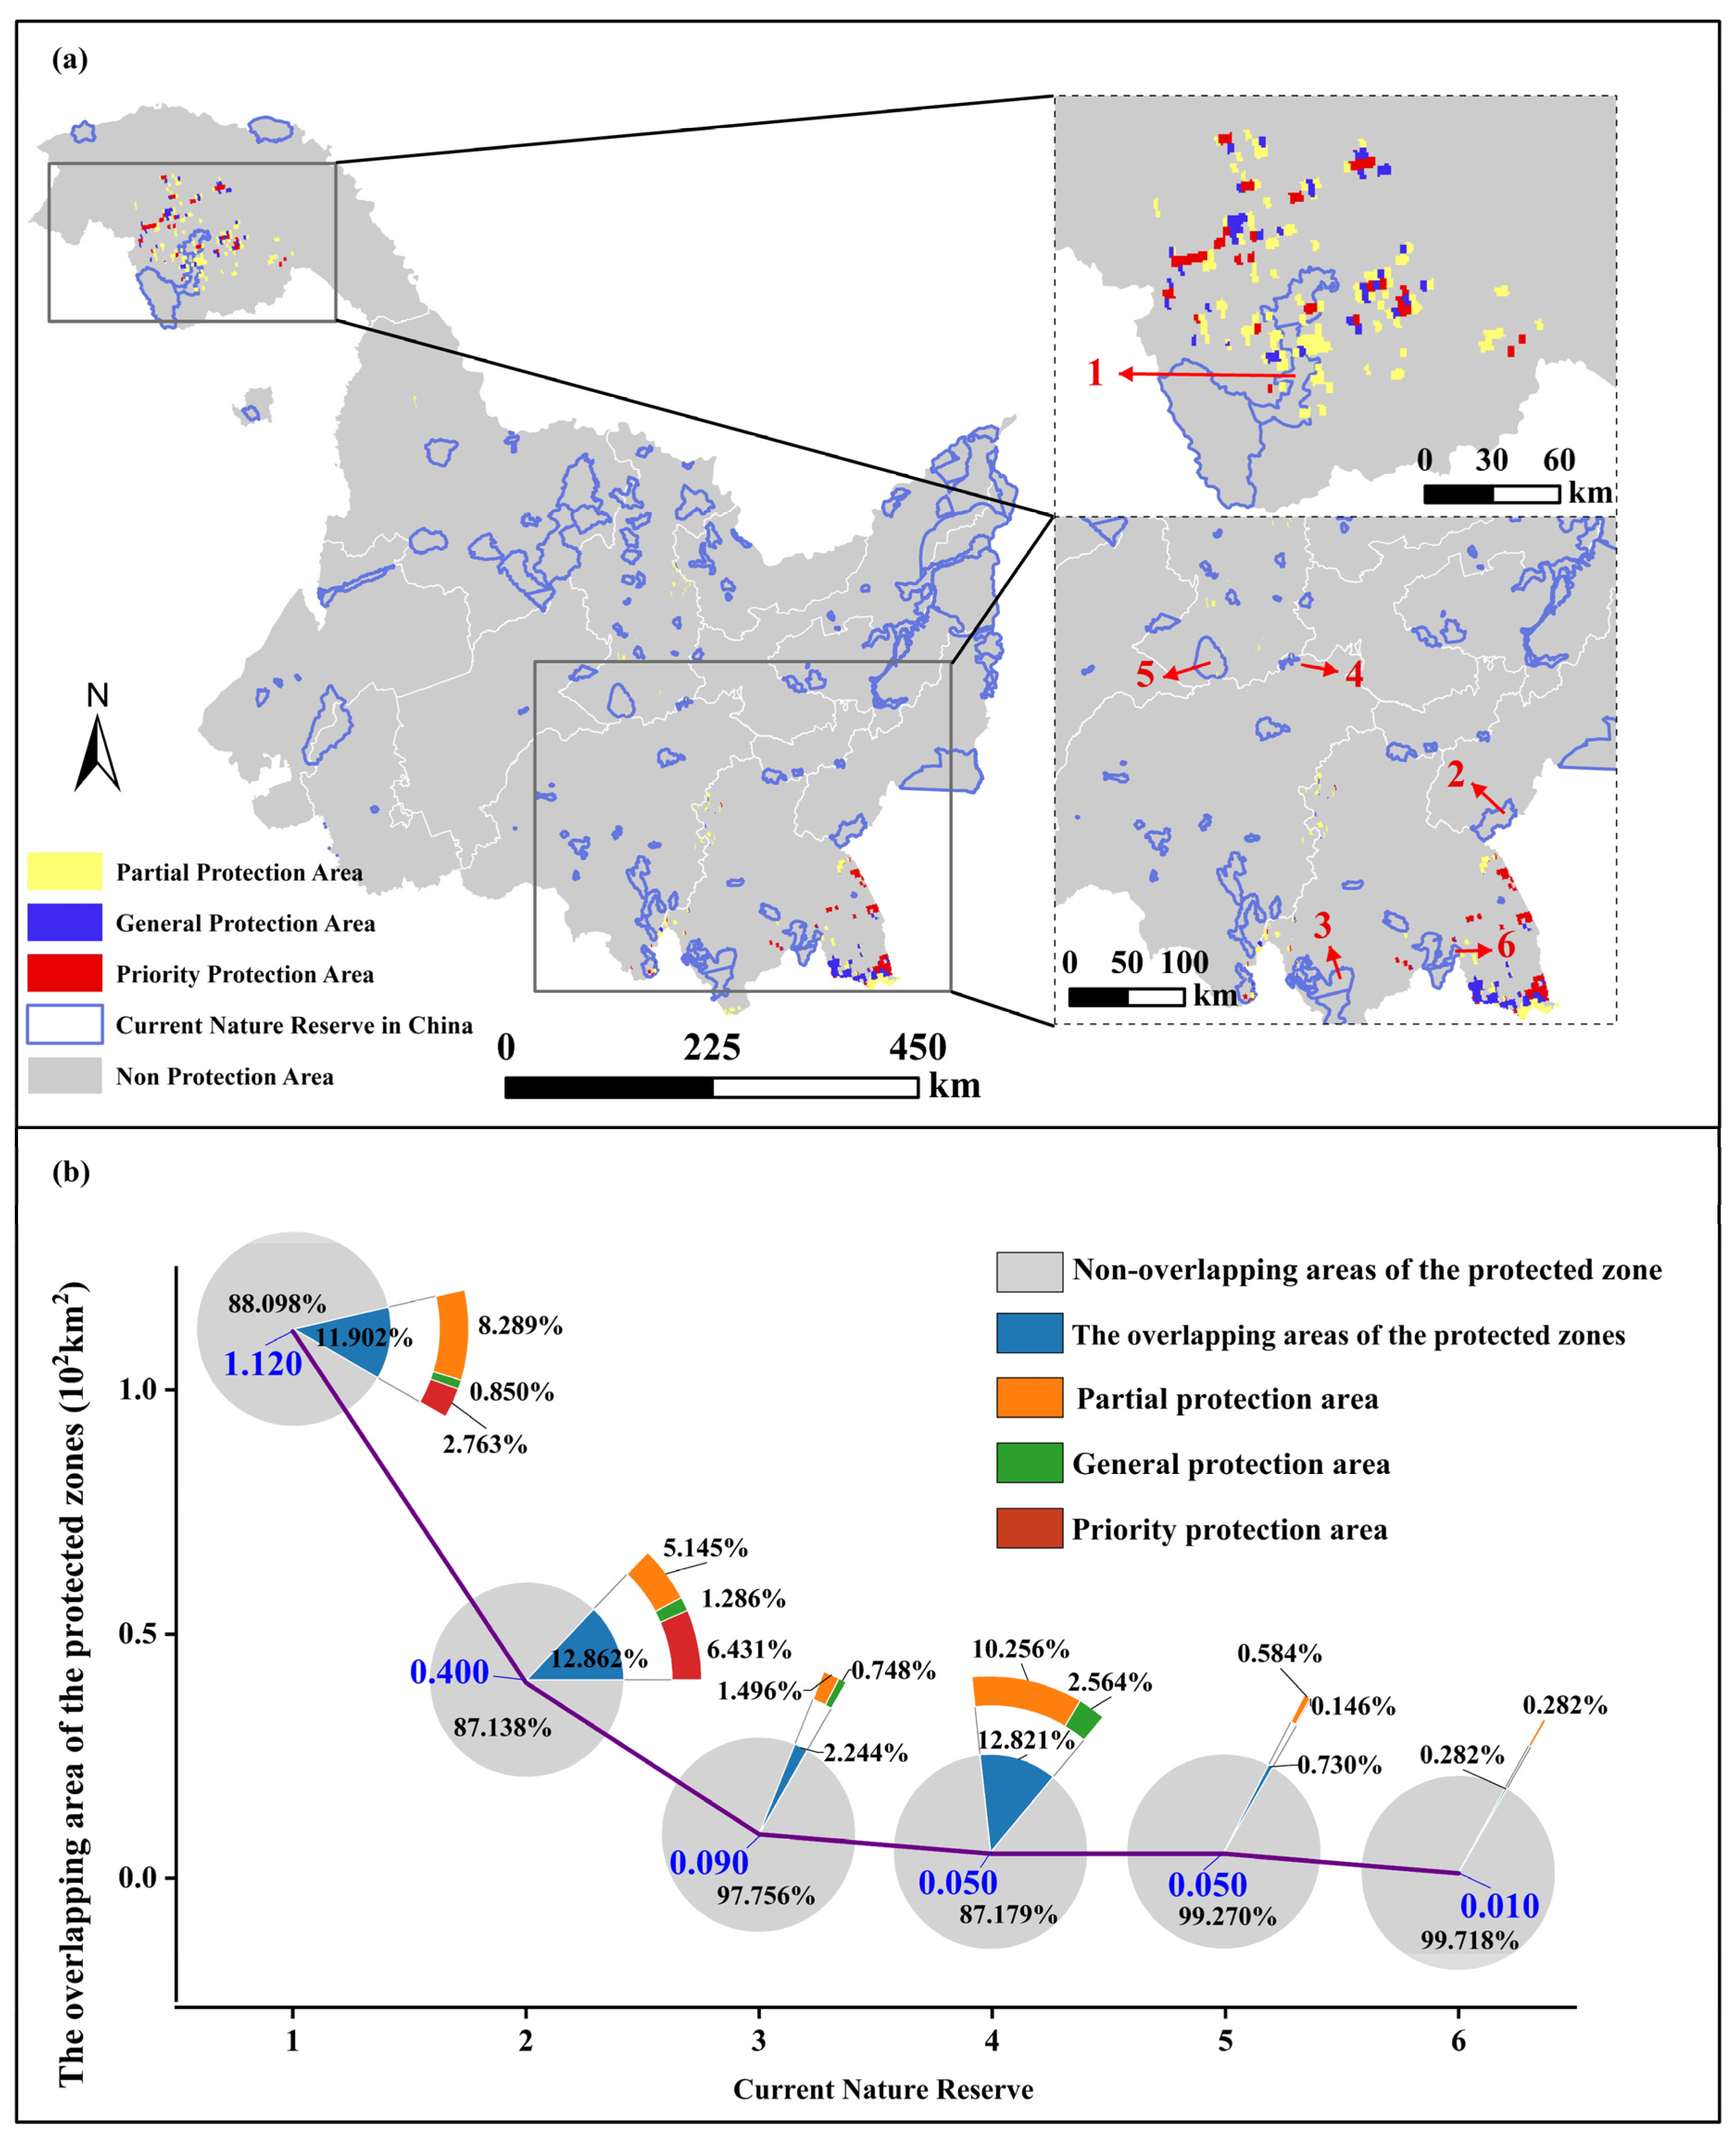
Against the background of future global climate change, the total area of the protected areas planned in Heilongjiang Province is 4.392 × 10³ km2, accounting for 20.00% of the stable naturally suitable habitat area, and is mainly distributed in the Greater Khingan Range and Laoyeling Range, with a small portion distributed in the Lesser Khingan Range. Among them, the area of priority protection zones is 1.098 × 10³ km2, the area of general protection zones is 1.098 × 10³ km2, and the area of partial protection zones is 2.196 × 10³ km2. Among the existing protected areas in Heilongjiang Province, there are six protected areas that overlap in area with the overall planned S. chinensis protection zones, which are Huzhong National Forest Park, Fenghuangshan National Forest Park, Heilongjiang Xiaobeihu Nature Reserve, Danqinghe National Forest Park, Xiaoxing’anling National Geopark in Yichun City, Heilongjiang Province, and Muling Taxus cuspidata National Nature Reserve. Among these overlapping protected areas, the overlapping area with the planned priority protected regions is 0.470 × 10² km2, accounting for only 4.281% of the total area of all priority protected areas. Specifically, the planned S. chinensis protected area within Huzhong National Forest Park is the largest, at approximately 1.120 × 10² km2, which constitutes 11.902% of the total area of Huzhong National Forest Park. Within this protected area, the priority protected zone covers 0.260 × 10² km2, the general protected zone covers 0.800 × 10² km2, and the partial protected zone covers 0.780 × 10² km2 (Figure 9).

3.6.2. Planning of Targeted Wild Tending Areas for S. chinensis in Heilongjiang Province Under Global Change

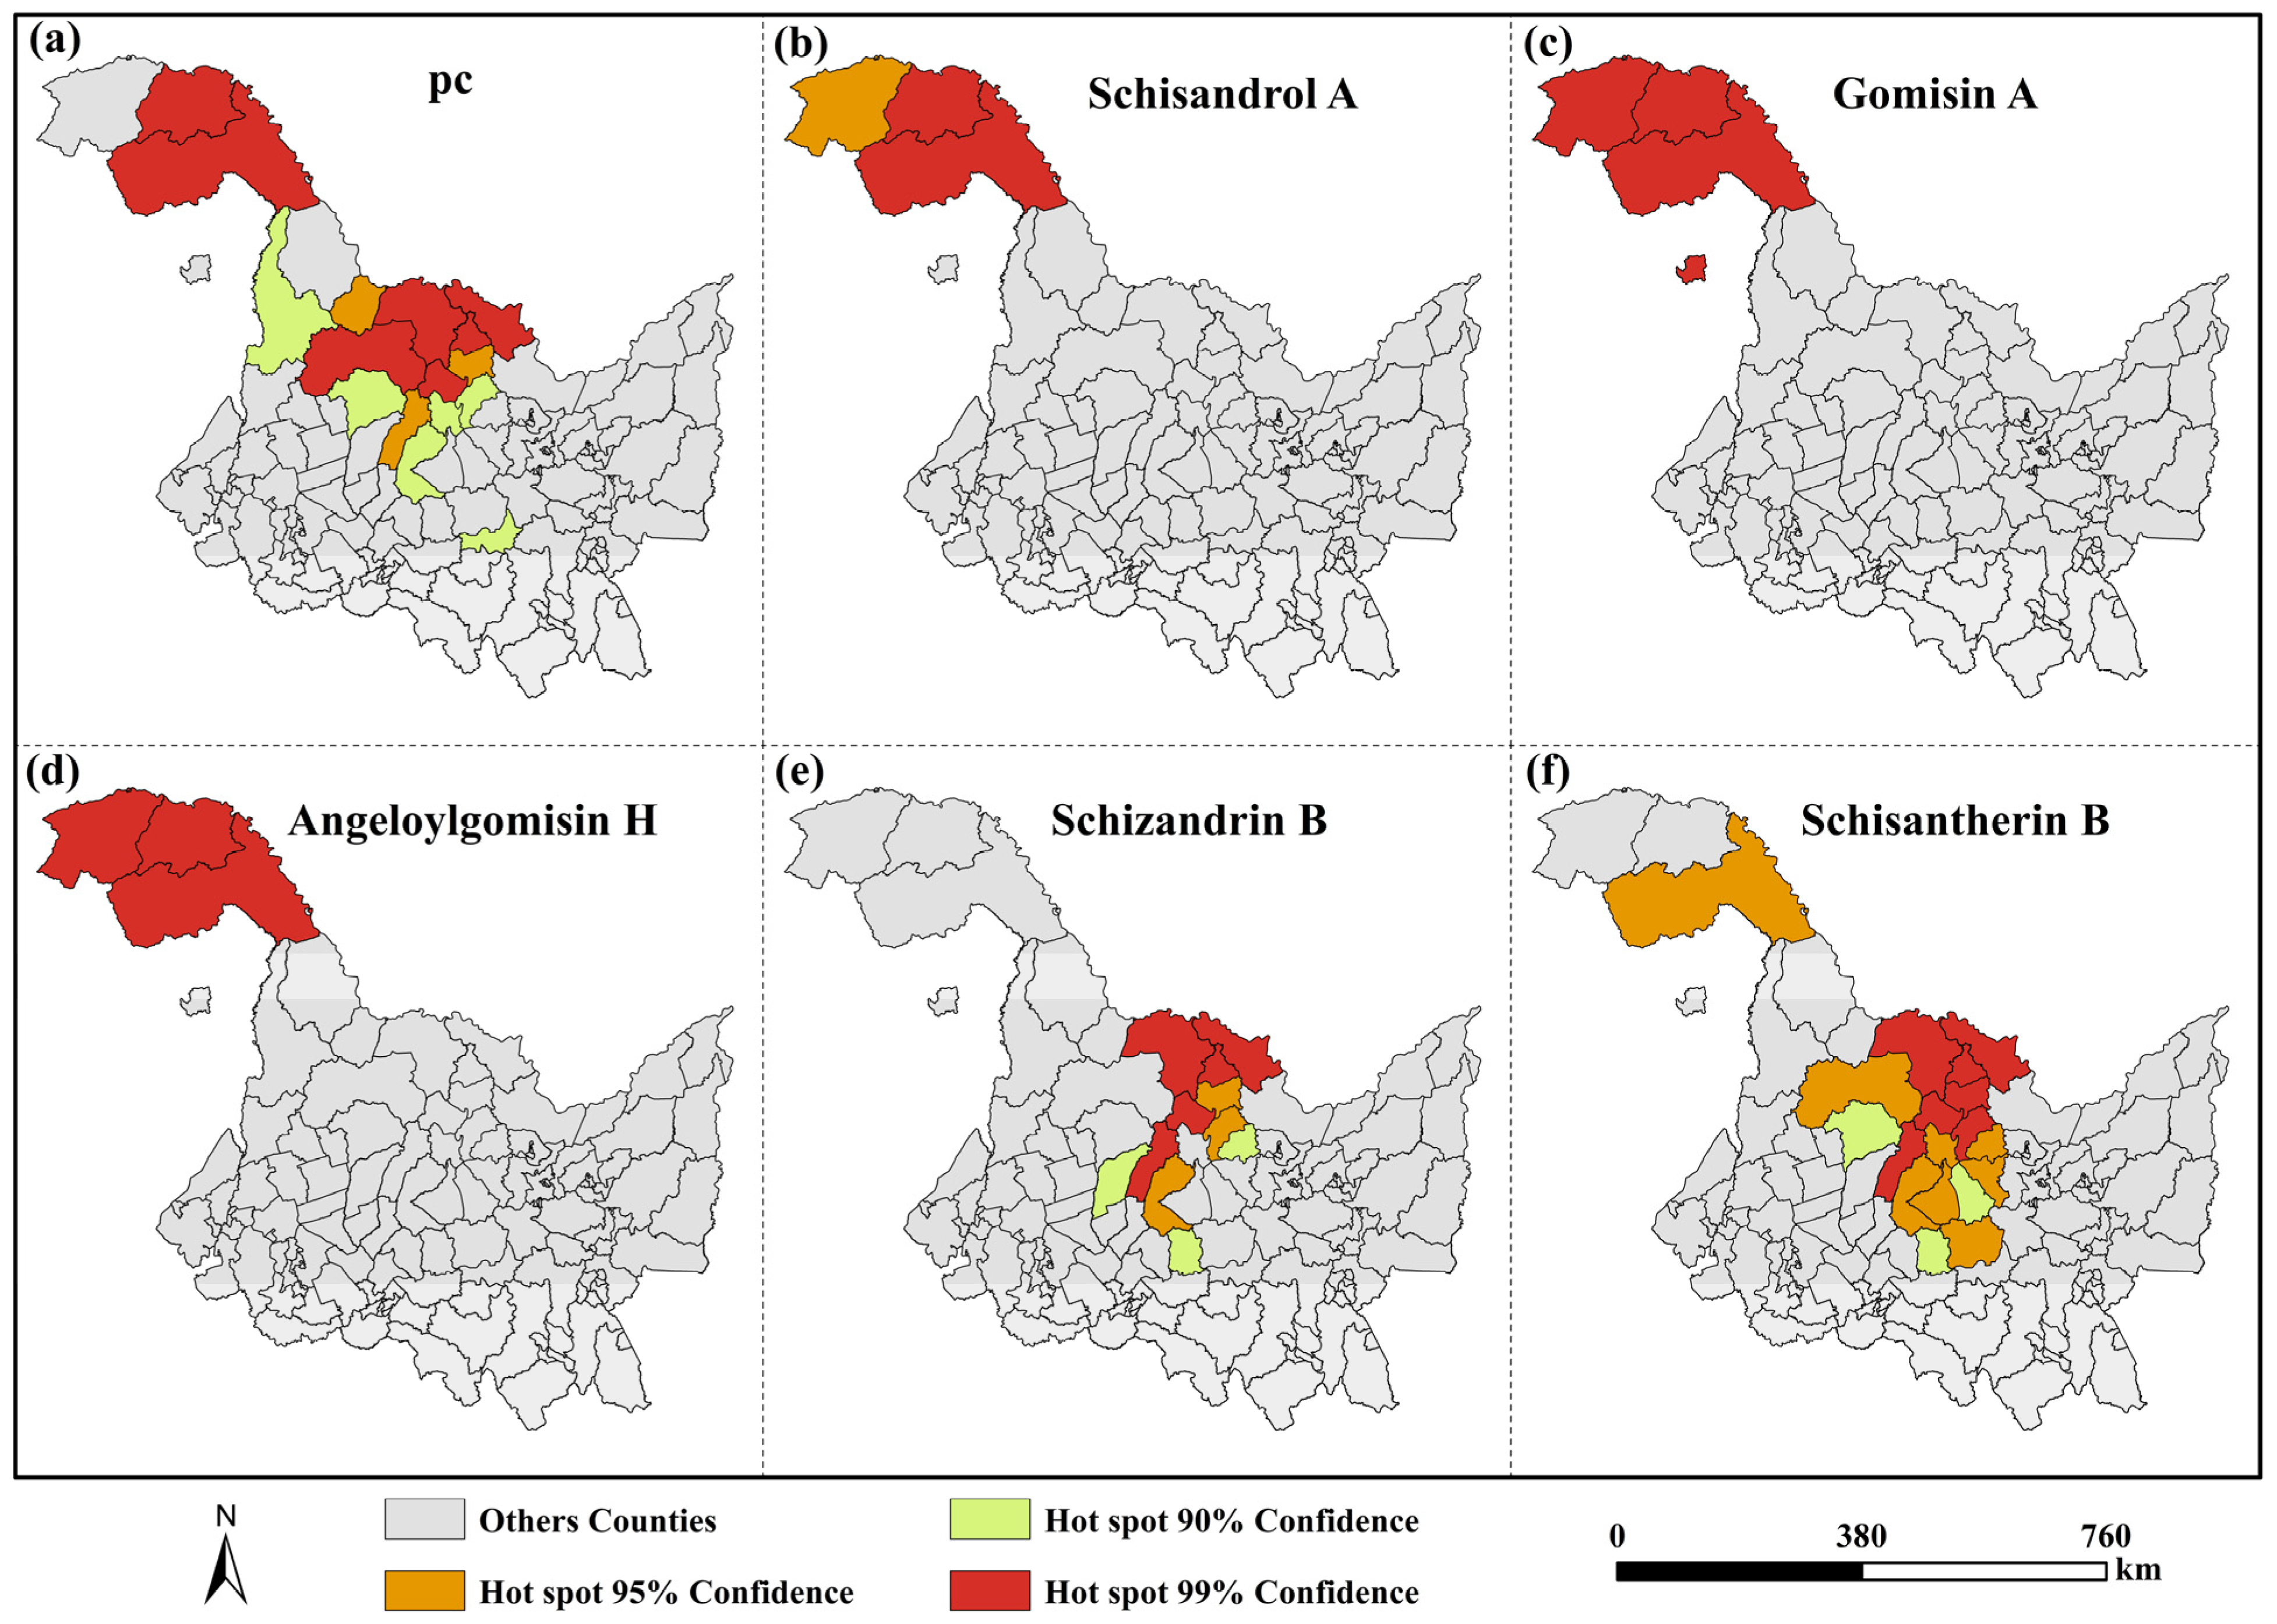
Under current climatic conditions, the Greater Khingan Range and Lesser Khingan Range are the most suitable regions for the development of wild tending of S. chinensis in Heilongjiang Province. Specifically, when targeting high-quality comprehensive components, Huma County and Tahe County in the Greater Khingan Range, multiple counties and districts in the Lesser Khingan Range, and Fangzheng County are hotspot regions for wild tending of S. chinensis; when targeting high content of high-quality Schisandrol A, Huma County, Tahe County and Mohe City in the Greater Khingan Range are hotspot regions for wild tending of S. chinensis; when targeting high content of high-quality Gomisin A, all four counties and districts (Huma County, Tahe County, Mohe City and Jiagedaqi District) in the Greater Khingan Range are hotspot regions for wild tending of S. chinensis; when targeting high content of high-quality Angeloylgomisin H, Huma County, Tahe County and Mohe City in the Greater Khingan Range are hotspot regions for wild tending of S. chinensis; when targeting high content of high-quality Schizandrin B, most counties and districts in the Lesser Khingan Range are hotspot regions for wild tending of S. chinensis; when targeting high content of high-quality Schisantherin B, most counties and districts in the Lesser Khingan Range are hotspot regions for wild tending of S. chinensis (Figure 10).
Under future global change scenarios, the hotspot counties suitable for wild tending of S. chinensis with high contents of the comprehensive components Schizandrin B and Schisantherin B show a trend of shifting toward the northwest, accompanied by a decrease in both quantity and hotspot intensity. With the passage of time and increasing carbon emissions, by the 2090s under the SSP5-8.5 scenario, it is projected that only Tahe County and Huma County in the Greater Khingan Range region of Heilongjiang Province will remain as hotspot areas. The hotspot counties suitable for wild tending of S. chinensis with high contents of Schisandrol A, Gomisin A and Angeloylgomisin H remain stable and are concentrated in the Greater Khingan Range region. However, with the passage of time and increasing carbon emissions, both the number of hotspot counties and hotspot intensity will also decrease by the 2090s under the SSP5-8.5 scenario (Figures S6–S11).

4. Discussion

4.1. Improvement and Application of Species Distribution Models in the Prediction of Suitable Areas for S. chinensis

Species distribution models (also known as ecological niche models or habitat suitability models) have become a common tool for addressing fundamental and applied issues related to biodiversity. Nevertheless, limitations of the core principles and standardized operational protocols of species distribution models are commonly observed in empirical research. These limitations are not only reflected in confusion about niche concepts (e.g., fundamental vs. realized niche), but also in the neglect of data quality issues, including species misidentification and collector bias. These factors significantly undermine the ecological validity of model outputs [66,67]. Furthermore, existing studies rely solely on occurrence records provided by open online databases such as GBIF, and fail to incorporate standardized field-collected survey data, which often results in biased prediction outputs [68]. Meanwhile, most regional-scale species distribution modeling still adopts a single algorithm, and does not effectively utilize ensemble modeling approaches such as Biomod2, which have been demonstrated to deliver higher robustness and prediction accuracy in comparative studies [69,70]. Most existing studies employ network-based data sources to simulate species distribution models at regional scales, typically using a single model for analysis [26,27,28,29,30]. Based on this, this study optimizes the prediction of the potential suitable areas for S. chinensis (Table 3). Firstly, relying on field investigations, basic databases and the plantR program package, this study constructed a relatively complete dataset of S. chinensis species distribution. Through data cleaning and quality control processes, erroneous and abnormal distribution points were eliminated, effectively improving the spatial coverage and prediction stability of the model. Secondly, based on the cleaned and screened valid occurrence points, this study delimits the distribution range of S. chinensis to the continental land area of Asia. According to the complete niche characteristics of the species at the Asian scale, this study constructs the potential suitable distribution area covering its entire climate domain, and then clips the prediction results to the study area (Heilongjiang Province). This strategy can effectively prevent the model from conducting unreasonable extrapolation beyond the range of training data when simulating future climate scenarios [71]. Finally, in terms of model algorithms, this study adopts the optimized ensemble model Biomod2, which effectively reduces the instability and systematic bias of a single model through multi-algorithm ensemble. Meanwhile, the Kuenm package is used to optimize the parameter configuration of the MaxEnt model, which avoids model overfitting and enables more accurate prediction of the dynamic changes in the suitable distribution areas of S. chinensis under different future climate scenarios [45,72].

4.2. Regulatory Effects of Key Environmental Factors on S. chinensis Growth

Based on the suitability area prediction results, the current suitable areas for S. chinensis are concentrated in the temperate regions of Northeast Asia, covering northeastern China, the Russian Far East, the Korean Peninsula, and parts of Japan. This region is dominated by a temperate monsoon climate, with climatic variations primarily influenced by meteorological factors such as the East Asian monsoon and tropical cyclones. It also exhibits transitional characteristics of a temperate continental climate. These characteristics include distinct seasons, concurrent rainfall and warmth, cold winters and warm summers, and uneven spatiotemporal distribution of precipitation. Such features align closely with S. chinensis’s ecological adaptability to light, moisture, and cold tolerance [34]. Wild S. chinensis naturally occurs in habitats such as forest edges and shrublands in mountain valleys, thriving at elevations between 1200 and 1700 m. Moreover, the complex and diverse topography of Northeast Asia, combined with high vegetation cover and rich plant communities, provides a wide range of altitudes, from sea level to 4880 m. This offers extensive and varied ecological niches for the survival and reproduction of S. chinensis [73,74,75].
Based on the simulation outputs from the Biomod2 model, the key environmental factors driving the growth of S. chinensis, ranked by the magnitude of their influence, are winter solar radiation (srad_winter), precipitation of the warmest quarter (bio18), summer solar radiation (srad_summer) and precipitation of the wettest month (bio13). This indicates that light availability and precipitation are the core environmental factors regulating the growth of S. chinensis. In this study, the influences of temperature and soil factors on the geographical distribution of S. chinensis were incorporated into model calculation. The results show that their contribution rates are significantly lower than those of precipitation climatic factors and solar radiation factors. It is inferred that although temperature is a critical environmental factor affecting plant distribution, it may have a high collinearity with solar radiation, and its contribution rate is lower than that of solar radiation; therefore, the model does not identify temperature as the dominant factor affecting the distribution of S. chinensis [76]. Meanwhile, although soil conditions are the necessary foundation for the growth of S. chinensis, they are not the dominant factor restricting its growth and distribution. This conclusion is consistent with the research findings reported by L [77].
For individual plants, the accumulation of appropriate light radiation is critical for initiating their life cycle, namely seed germination, seedling growth and flowering [78]. S. chinensis is a climbing vine plant. Climbing plants feature a high light saturation point, which is reached when the light level is close to the higher light intensity of the habitat. This trait ensures that a relatively high photosynthetic rate can be maintained throughout the entire lifespan of the leaves. In addition to a high light saturation point, climbing plants also possess a low light compensation point, and many species growing under high light conditions exhibit a low light compensation point [79]. Since plants cannot accumulate dry matter at the light compensation point, the level of this point is significant for determining whether plants can thrive under low light intensity [80]. S. chinensis, as a sun-loving yet shade-tolerant plant, relies heavily on light for its growth. Being a monoecious species, light plays a crucial regulatory role in the differentiation of male and female flowers in S. chinensis. Li et al. found that S. chinensis growing in open areas and forest edges flower earlier than those in the forest interior, with fruit ripening occurring 4–7 days earlier as well; furthermore, the proportion of female flowers in wild northern S. chinensis shows an increasing trend from forest interior to forest edge to open areas [81]. The differentiation of male and female flowers in S. chinensis begins in late July, reaching its peak during mid- to late August, indicating that suitable light conditions in summer significantly influence the plant’s fruiting capacity [82]. In mid- to high-latitude regions of the Northern Hemisphere (40–90° N), solar radiation accumulates over a period of 1–3 months without lag, so winter solar radiation can promote shoot regreening and bud break in S. chinensis [78,82]. Under global warming, the combination of rising winter temperatures and abnormal short photoperiods can lead to premature deacclimation of trees and reduced frost resistance. This, in turn, limits plant distribution to some extent, because subsequent cold snaps or late frosts can cause frost damage [83].
Precipitation regulates plant growth by influencing physiological processes, soil moisture, and nutrient availability [84]. S. chinensis is a climbing plant with well-developed root systems that can efficiently utilize soil water [85]. When precipitation decreases, plants allocate more biomass to roots to enhance water uptake [86]. Under such conditions, S. chinensis may adopt a differential response strategy, characterized by increased root biomass while aboveground growth is correspondingly suppressed [87]. In contrast, high precipitation can enhance soil nitrogen mineralization and plant nitrogen use efficiency, thereby increasing total plant biomass [88]. However, excessive rainfall leads to soil saturation, which reduces the partial pressure of oxygen around plant roots. This typically decreases root permeability, limiting water uptake. Thus, despite ample moisture in the soil, plants may still experience water deficit [89]. As a monoecious plant, the differentiation of male and female flowers in S. chinensis is also influenced by precipitation. Zhao et al. hypothesized that, according to resource allocation theory, drought in the previous year could lead to adjustments in sex expression of S. chinensis, specifically a decrease in the proportion of female flowers [90]. This study shows that the suitable growing regions for S. chinensis are concentrated in temperate northeastern Asia, where the wettest month and warmest season coincide with summer. Concentrated summer rainfall can cause abnormal physiological metabolism in S. chinensis, often resulting in flower and fruit drop [91]. Moreover, Seo et al.’s research indicated that excessive precipitation increases soil moisture content, leading to reduced photosynthetic and transpiration rates in S. chinensis [92].

4.3. Spatiotemporal Migration Patterns and Survival Risk Assessment of S. chinensis Habitats in Heilongjiang Province Under Global Change

The coupled mechanisms of climate change, species’ ecological adaptability, and land use changes jointly determine the future spatiotemporal evolution patterns and dynamic distribution characteristics of S. chinensis habitats in Heilongjiang Province [18]. Under future climate change scenarios, S. chinensis responds to climatic stress by shifting its habitat spatially and temporally. This response is driven by its ecological niche characteristics. These include temperature and humidity adaptability, soil preferences, and phenological rhythms. Meanwhile, land use exerts an additive disturbance effect on this habitat migration process through landscape pattern restructuring and changes in habitat connectivity. The results show that under the low-emission SSP1-2.6 scenario, the habitat area of S. chinensis remains dynamically stable overall. This is closely related to the fact that regional temperature rise in this scenario is kept below 2.0 °C and precipitation patterns remain relatively stable, resulting in no significant shift in the species’ habitat range. The species can gradually adapt to mild climate change through its own ecological plasticity [93,94]. Under the SSP2-4.5, SSP3-7.0 and SSP5-8.5 carbon emission scenarios, the area of S. chinensis habitats in Heilongjiang Province shows a gradual decreasing trend over time, and the suitable habitats are gradually shifting to the Greater Khingan Range region in the northwest direction. As a typical temperate deciduous woody vine, the growth and development of S. chinensis has a strict adaptive requirement for humidity thresholds [82]. Under the medium-high emission scenario, alterations in precipitation patterns have intensified the aridity degree in Heilongjiang Province. S. chinensis features shallow root systems and prefers moist, fertile soils with a pH value ranging from 5.5 to 7.0. Only sufficient water supply during the growing season can promote its growth, flowering and fruit set, while soil water deficit will further exacerbate the unsuitability of habitats [34,95]. In contrast, the Greater Khingan Range region, influenced by monsoon circulation and topographic lifting, has more uniform precipitation distribution. Furthermore, the humus layer formed by the decomposition of coniferous forest litter can effectively maintain soil moisture, which meets the soil ecological requirements of S. chinensis [96,97].
Land use changes may damage species habitats and the connectivity between them, preventing species from dispersing from their current habitats to future suitable habitats, which in turn increases the risk of species extinction [98]. It is projected that by 2050, 10% to 20% of natural grasslands and forests will be replaced by agricultural and urban infrastructure [99]. The reduction in forest area will result in a lack of climbing attachment substrates for wild S. chinensis, exerting adverse impacts on the growth of this species. Putz et al. noted that the population density of climbing plants will decline over time when they lack adequate attachment substrates [100]. The flowering and fruiting rate of S. chinensis is closely correlated with light conditions, thus this species generally exhibits a higher fruiting rate in forest edge habitats [81]. However, land use change inevitably leads to the reduction in forest area in the natural habitats of S. chinensis, and the forest edge zones suitable for its flowering and fruiting are the first to be damaged, which severely threatens the survival of S. chinensis populations [101]. In conclusion, under the combined pressure of future climate change and land use change, the area of suitable habitats for S. chinensis in Heilongjiang Province will inevitably shrink, and its spatial distribution centroid is projected to migrate to the Greater Khingan Range forest area in the northwest direction. This result indicates that the current conservation system located in southeastern Heilongjiang will face the risk of failure, and future conservation planning should be expanded to the Greater Khingan Range region, while strengthening the management and control of land use along the migration corridors.

4.4. Spatial Response Characteristics and Environmental Driving Mechanisms of the Chemical Constituents of S. chinensis in Heilongjiang Province

In this study, the main secondary metabolites of S. chinensis were determined, including Schisandrol A, Gomisin A, Angeloylgomisin H, Schizandrin B, Schisantherin B and Schizandrin A. All of these metabolites are lignans, which belong to phenylpropanoids, and their biosynthesis is initiated via the phenylpropanoid metabolic pathway [102]. With the exception of Schizandrin A, the contents of all other components exhibited significant responses to environmental factors, and the spatial response patterns of different components showed obvious differentiation. This difference may be closely associated with their respective metabolic branches and regulatory mechanisms.
The results of all-subsets regression show that the lignin content of S. chinensis in this study is correlated with temperature, precipitation, soil properties, solar radiation and other environmental factors. Among these factors, lignin content exhibits a significant positive correlation with temperature factors. Existing studies have demonstrated that high temperature can activate the glycolysis pathway of S. chinensis, thereby increasing the content of phenylalanine. As a precursor substrate for lignin biosynthesis in S. chinensis, the accumulation of phenylalanine will further promote lignin synthesis in S. chinensis [103]. Excessive precipitation inhibits lignin accumulation in S. chinensis. Under normal circumstances, drought stress suppresses the physiological processes of numerous plant species, thereby hindering their growth and development [104]. Nevertheless, plants have evolved drought adaptation mechanisms mediated by the phenylpropanoid biosynthetic pathway [105]. Earlier studies have demonstrated that up-regulated expression of flavanone 3-hydroxylase (F3H), phenylalanine ammonia-lyase (PAL), 4-coumarate-CoA ligase (4CL) and flavonol synthase (FLS) can enhance plant drought tolerance; furthermore, elevated activity of PAL and 4CL also promotes lignin biosynthesis [102,106]. This study reveals that the content of Gomisin A is negatively correlated with bio14 (precipitation of the driest month), indicating that moderate drought stress facilitates the accumulation of Gomisin A. Studies conducted by Ri et al. demonstrate that moderate UV-B radiation can induce S. chinensis to activate stress resistance mechanisms and promote the accumulation of stress-resistant secondary metabolites such as lignin; however, excessive UV-B radiation inhibits the accumulation of certain key stress-resistant secondary metabolites, such as the phenolic compound 4-hydroxycinnamic acid. 4-hydroxycinnamic acid, as a precursor for lignin biosynthesis in S. chinensis, leads to a reduction in lignin synthesis when its content decreases [102,107,108]. This result is consistent with the conclusion obtained in this study that excessive summer solar radiation inhibits the accumulation of partial lignin in S. chinensis. Different from the monotonic effects of temperature, precipitation and solar radiation on the lignin accumulation in S. chinensis, the regulatory effect of soil factors is more complex. Since it involves multiple aspects including pH, cation exchange capacity and soil texture, its impact on lignin accumulation exhibits multi-directionality and heterogeneity. The stronger the cation exchange capacity (CEC) of clay soil, the more effectively it can retain and supply cation nutrients required by plants (e.g., K+). An increase in K+ content can raise the content of lignin monomers, thereby providing a material basis for the synthesis of S. chinensis lignin [109]. In contrast, across a broader range of soil types, CEC exhibits a negative correlation with the lignin content of S. chinensis. We hypothesize that this phenomenon is primarily associated with soil texture. Loam and sand show a negative correlation with CEC. They generally have favorable drainage without waterlogging, but are prone to intermittent drought, and this drought promotes secondary metabolism. On the other hand, an excessive increase in CEC, especially when induced by very high clay content, tends to worsen soil aeration and hydraulic conductivity [110,111,112,113,114]. This extreme physical edaphic environment restricts root activity, and is thus unfavorable for the accumulation of plant secondary metabolites [115]. Soil pH influences the lignin content in S. chinensis. It is hypothesized that soil pH indirectly mediates the regulation of lignin biosynthesis in S. chinensis via rhizosphere microorganisms, such as Arthrobacter and Paenibacillus [116]. This study demonstrates that the volume percentage of gravel in topsoil (t_gravel) is negatively correlated with lignin accumulation in S. chinensis. An increase in soil gravel content reduces the available water and nutrient contents in topsoil [117]. To adapt to such resource limitations, plants typically promote root growth into deeper soil layers to acquire water and nutrients [118]. During this process, water stress can induce increased lignin synthesis and deposition in roots, which is manifested as enhanced root lignification [119]. Based on the theoretical hypothesis of carbon allocation trade-off [120], this process may lead to a reduction in lignin allocated to other organs, such as fruits. However, there is currently no direct experimental evidence to support this inference, and further research is required to verify it.

4.5. Conservation and Utilization of S. chinensis in Heilongjiang Province Under Global Change: Challenges and Countermeasures

The ability of a population to adapt to climate change depends, to a certain extent, on the average lifespan of individuals and their age at reproductive maturity [121]. As a tree species with long generation time and lifespan, S. chinensis has a weaker capacity than annual plants to establish new genotypes and adapt to rapid climate change. Furthermore, field investigations reveal that although S. chinensis is widely distributed across forests, it almost fails to flower and fruit in environments with high canopy closure, and relies primarily on subterranean rhizomes for asexual reproduction. This trait weakens the ability of S. chinensis to generate new genotypes, and in turn reduces its adaptability to rapid climate change. Meanwhile, due to anthropogenic activities including agricultural expansion, timber harvesting, infrastructure construction and urbanization, the forest habitats that S. chinensis depends on for survival will be subjected to tremendous pressure [122]. Furthermore, as a significant genuine medicinal material in Heilongjiang Province, S. chinensis has extremely high medicinal value. However, driven by economic interests, some pickers adopt destructive harvesting methods such as cutting vines and felling trees to obtain temporary convenience during fruit collection, engaging in predatory exploitation [123]. This behavior has caused severe damage to wild S. chinensis resources, resulting in a sharp decline that is of great concern and urgently requires high-level attention. Accordingly, this study comprehensively incorporates two core driving factors, namely climate change and land use change, and systematically delineates priority conservation areas for S. chinensis in Heilongjiang Province, with the aim of providing urgently needed theoretical basis for government departments to formulate resource conservation strategies for S. chinensis. All protected areas planned in this study are forest habitats that can maintain climate suitability by the end of this century, interference zones such as residential areas and cultivated land were excluded. On the basis of Zonation prioritization ranking, we set the conservation target as the top 20% of high-priority grid cells. Existing literature shows that protecting 5–20% of high-quality habitats can cover the core populations of more than half of the target species. Therefore, this threshold has sufficient basis for biodiversity conservation, while avoiding land conflicts caused by blind boundary expansion, and is feasible in practical operation [124]. In addition, we applied Zonation to protected area planning in this study. The algorithm itself embeds spatial proximity weights during the iterative removal process, so that the preferentially retained grid cells naturally tend to be aggregated in distribution rather than forming scattered patches. This ensures that the selected sites can support the migration and gene flow of S. chinensis populations under the background of climate change [125].
The results show that although the current suitable habitats of S. chinensis already cover some national and provincial nature reserves, under future climate change scenarios, existing nature reserves only cover 4.28% of the total area of priority conservation areas. A large number of high-conservation-value areas have not yet been incorporated into the conservation system, resulting in a significant conservation gap. Among existing protected areas, Huzhong National Forest Park has the largest area of priority conservation zones. Its spatial units provide highly suitable climatic conditions for S. chinensis growth, and the region’s climate is expected to remain relatively stable over the next century, minimizing potential impacts of climate change on S. chinensis populations. Additionally, Fenghuangshan National Forest Park, Xiaobeihu Nature Reserve in Heilongjiang, Danqinghe National Forest Park, Xiao Xing’anling National Geopark in Yichun City, Heilongjiang Province, and Muling Taxus cuspidata National Nature Reserve can also contribute to the conservation of S. chinensis in Heilongjiang Province. Based on the aforementioned characteristics, Huzhong National Forest Park is expected to become the core region for the conservation of S. chinensis within this century, providing critical support for the population maintenance and long-term persistence of this species. Meanwhile, we recommend establishing monitoring sites in areas with dense S. chinensis populations within the six protected areas that exhibit a large overlapping area with the planned protected areas, and conducting regular assessments of the population distribution dynamics. This will ensure that the population size in climatically stable regions remains unaffected by other external disturbances, and facilitate the timely development of adaptive management measures. In addition, we recommend that district- and county-level governments guide the establishment of provincial-level germplasm resource protection bases for S. chinensis. This recommendation specifically targets protection gap areas, such as the Greater Khingan Range region and the Laoye Range region, where such gaps are large. Such bases should implement in situ conservation for native populations to stabilize community structure and maintain genetic diversity. In addition, they should systematically collect excellent local germplasm resources and conduct experiments on seedling propagation, population scale expansion, and wild tending. The ultimate goal is to gradually expand population size and restore degraded habitats.
In addition to protecting wild S. chinensis resources, artificial cultivation has become an important approach to supply S. chinensis medicinal materials to meet the growing demand of the medical market. Against the background of the policies of “non-grain cultivation” and “non-agricultural utilization” of cultivated land, the understory wild tending mode, which does not occupy cultivated land resources, has become an effective way to alleviate the supply pressure of S. chinensis medicinal materials. In this study, when planning the wild tending areas for S. chinensis in Heilongjiang Province, global change and the demand for different active components of S. chinensis were comprehensively considered, and targeted wild tending areas that balance adaptability to global change and meet the demand for multiple components were constructed. The planned areas can not only ensure that the climatic conditions remain continuously suitable for the growth of S. chinensis throughout this century, but also directionally provide a variety of high-quality S. chinensis components in response to different market demands. Meanwhile, this study provides a reference for the commercial cultivation of S. chinensis, thereby alleviating the shortage of wild S. chinensis resources to the maximum extent. According to the planning, Tahe County and Huma County in the Greater Khingan Range region are delimited as the most suitable areas for wild tending of S. chinensis. This region can guarantee a continuous and stable supply of high-quality S. chinensis medicinal materials throughout this century. Based on the planning results, we put forward the following recommendations: (1) Wild tending of S. chinensis is concentrated in hotspots such as Tahe County and Huma County. In these areas, local governments should be guided to formulate targeted policies and provide supportive measures including technical guidance for tending, so as to encourage enterprises and individuals to conduct commercial simulated wild cultivation. This measure can not only reduce the consumption of wild resources through artificial field cultivation and alleviate the pressure on the supply of medicinal materials, but also promote the population proliferation and habitat restoration of S. chinensis through human intervention. (2) Priority should be given to the systematic collection and ex situ conservation of high-quality S. chinensis germplasm resources in regions such as the Greater Khingan Range. Excellent germplasm resources from different geographical origins with significant differences in active ingredient content shall be extensively collected. Meanwhile, efforts shall be made to promote the breeding and large-scale propagation of improved varieties, so as to provide high-quality germplasm foundation for the recovery of wild populations and the development of industrial cultivation.

5. Conclusions

Against the background of global change, this study constructs suitable habitats for S. chinensis in Heilongjiang Province under climate stabilization scenarios based on climate change and land use change. Combined with the scope of current protected areas, this research systematically identifies existing conservation gaps and scientifically plans priority protected areas for S. chinensis in Heilongjiang Province. On this basis, combined with high-performance liquid chromatography and principal component analysis, this study accurately identifies the high-quality spatial distribution of various components of S. chinensis through all-subsets regression analysis, and ultimately identifies the core hotspot counties for wild tending of S. chinensis in Heilongjiang Province. Although some scholars currently question the prediction results of species distribution models, this study holds that as long as we build on the basis of accurate and comprehensive species distribution data, systematically integrate multi-dimensional influencing factors such as climate change and land use pattern change, and further optimize the screening scheme for model parameters and environmental variables, the prediction results of the model still have important academic reference value and practical guiding significance. In conclusion, this study lays a solid scientific theoretical foundation for the conservation and directed cultivation planning of wild S. chinensis populations in Heilongjiang Province, and can provide accurate and scientific technical guidance for wild tending practices conducted by local forestry authorities and relevant industrial entities. Accordingly, it can effectively improve the quality and efficiency of S. chinensis resource cultivation and facilitate the high-quality development of the traditional Chinese medicine characteristic industry. In addition, the optimized approach proposed in this study for integrating multi-dimensional impact factors into species distribution models also provides a practical methodological reference for subsequent habitat suitability assessment and sustainable resource utilization planning of similar endangered medicinal plants.

6. Limitations and Future Research Directions

This study has several limitations. (1) When constructing the assessment of future habitat suitability, this study only adopts forest distribution change as a surrogate indicator of land use change, and does not incorporate such ecological factors as forest quality, habitat fragmentation, canopy structure, disturbance intensity and the differences between natural forests and planted forests. This may introduce certain biases into the estimation of the future habitat availability of S. chinensis. (2) It is noteworthy that since the present study aims to elucidate the correlation between the spatial distribution of medicinal component contents and environmental factors, the regression model of chemical components constructed for spatial prediction has not been validated. Accordingly, the research results only provide reference value for the selection of the optimal regression model in this study, and there are certain limitations regarding the validity of the prediction. (3) This study only addresses the correlation between the content of medicinal components in S. chinensis and external abiotic environment; however, the medicinal quality of S. chinensis may also be affected by factors such as genetic variation and soil microorganisms. In response to the above limitations, future research will be conducted from the following perspectives: (1) At the level of habitat suitability assessment, although the current practice of using forest distribution as a substitute for land use change is feasible, it obviously simplifies the heterogeneity of forest habitats. In the next step, we plan to integrate multi-source remote sensing and ground plot data, incorporate stand canopy density, edge effect index, vertical canopy structure parameters and disturbance history into the model, and distinguish the functional differences between natural secondary forests and pure planted forests in providing habitat resources. (2) In response to the limitations of the present study regarding the validity validation of regression models, future research will address these deficiencies from the following aspects: strategies including cross-validation, external validation with independent samples, and leave-one-out cross-validation will be introduced to systematically evaluate the predictive performance of the selected model on sample points that are not involved in model construction, so as to improve the accuracy and credibility of model prediction. In addition, future research will continue to conduct supplementary field sampling in other regions, further enrich the sample collection from different regions, and enhance the practical application significance of the model in large-scale research. Through the establishment of the above multi-layer validation system, this study expects to ensure the rigor of prediction while providing more solid theoretical support for the correlation analysis between the spatial distribution of medicinal components and environmental factors. (3) Regarding the quality formation mechanism, the current research only focuses on the statistical correlation of abiotic environmental factors, which is still insufficient to reveal the regulatory network of the accumulation of medicinal components. Future research should clarify the genetic differentiation level of populations in different distribution areas, synchronously collect rhizosphere soil samples for metagenomic sequencing, and analyze the coupling relationship between core microbial groups (e.g., mycorrhizal fungi, nitrogen-fixing bacteria) and the lignan biosynthesis pathway. On this basis, we will distinguish the relative contributions of genetic background, soil biota and abiotic environment to quality traits, so as to provide a more causal-based discrimination framework for the zoning of high-quality medicinal materials.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/biology15171501/s1, Figure S1: Results of principal component analysis (PCA); Figure S2: Model assessment results of the main environmental factors; Figure S3: (a) The area of each suitable habitat for S. chinensis in the full ecological zone (Asia); (b) The suitable habitat areas for various grades of S. chinensis in Asian countries; (c) The suitable habitat areas for various grades of S. chinensis in Chinese provinces; (d) The suitable habitat areas for various grades of S. chinensis in cities of Heilongjiang Province; Figure S4: Future changes in key environmental factors; Figure S5: Similarity of S. Chinensis from 46 batches in Heilongjiang Province; Figure S6: Distribution of high-quality comprehensive constituents (pc) hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Figure S7: Distribution of high-quality Schisandrol A hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Figure S8: Distribution of high-quality Gomisin A hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Figure S9: Distribution of high-quality Angeloylgomisin H hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Figure S10: Distribution of high-quality Schizandrin B hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Figure S11: Distribution of high-quality Schisantherin B hotspot counties for wild tending of S. chinensis in Heilongjiang Province under future global change; Table S1: Environment variables used in MaxEnt model; Table S2: Initial result of MaxEnt model; Table S3: Correlation analysis of environmental factors (Percent contribution > 0%,Correlation coefficient |r| ≤ 0.8); Table S4: TSS values of individual models in Biomod2; Table S5: Ranking of environmental factors based on XGBoost-SHAP analysis; Table S6: Environmental factors in full subset regression; Table S7: Average values of main environmental factors, 95th percentile, minimum value and maximum value; Table S8: Changes in the suitable habitat of S. chinensis in Heilongjiang Province under different future shared socioeconomic pathway scenarios; The materials and methods employed for fingerprinting are also presented in the Supplementary materials (Supporting Information of The Chromatographic Fingerprint) [126,127,128].

Author Contributions

D.D. contributed to writing—original draft, software, methodology, and data curation. M.Y. provided supervision, writing—review & editing, and validation. M.L. undertook writing—review & editing, conceptualization and investigation. X.L. contributed to writing—original draft, formal analysis and software. H.X. performed writing—review & editing, investigation and validation. B.Z. was involved in writing—review & editing, supervision, methodology, and funding acquisition. X.Z. undertook writing—review & editing, supervision, resources, and funding acquisition. All authors have read and agreed to the published version of the manuscript.

Funding

This study was supported by Department of Science and Technology of Heilongjiang Province (XQ2026C036) and Education Department of Heilongjiang Province (LJYXLZR2025-074).

Institutional Review Board Statement

Not applicable.

Informed Consent Statement

Not applicable.

Data Availability Statement

The original contributions presented in this study are included in the article/Supplementary Materials. Further inquiries can be directed to the corresponding authors.

Acknowledgments

We thank Chen Wang (Harbin Normal University) for his assistance in identifying S. chinensis specimens. We also acknowledge financial support from the projects: “Collection, Evaluation, and Superior Strain Selection of High-Quality Germplasm Resources of Wild Schisandra chinensis in Heilongjiang Province” (XQ2026C036) and “Study on Protection Gap Identification and Wild Tending Regionalization of S. chinensis in Heilongjiang Province Based on ‘Ecology-Component’ Coupling” (LJYXLZR2025-074).

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Sen, T.; Samanta, S.K. Medicinal Plants, Human Health and Biodiversity: A Broad Review. In Biotechnological Applications of Biodiversity; Mukherjee, J., Ed.; Advances in Biochemical Engineering/Biotechnology; Springer: Berlin/Heidelberg, Germany, 2014; Volume 147, pp. 59–110. [Google Scholar]
  2. Farnsworth, N.R.; Soejarto, D.D. Global Importance of Medicinal Plants. In Conservation of Medicinal Plants; Akerele, O., Heywood, V., Synge, H., Eds.; Cambridge University Press: Cambridge, UK, 1991; pp. 25–52. [Google Scholar]
  3. Hamilton, A.C. Medicinal Plants, Conservation and Livelihoods. Biodivers. Conserv. 2004, 13, 1477–1517. [Google Scholar] [CrossRef] [Scilit]
  4. Bhattacharya, P.; Prasad, R.; Bhattacharyya, R.; Asokan, A. Towards Certification of Wild Medicinal and Aromatic Plants in Four Indian States. Unasylva 2008, 59, 35–44. [Google Scholar]
  5. Kling, J. Protecting Medicine’s Wild Pharmacy. Nat. Plants 2016, 2, 16064. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  6. Chen, S.; Yu, H.; Luo, H.; Wu, Q.; Li, C.; Steinmetz, A. Conservation and Sustainable Use of Medicinal Plants: Problems, Progress, and Prospects. Chin. Med. 2016, 11, 37. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  7. Liu, C.; Yu, H.; Chen, S. Framework for Sustainable Use of Medicinal Plants in China. Plant Divers. Resour. 2011, 33, 65–68. [Google Scholar]
  8. Huang, H. Plant Diversity and Conservation in China: Planning a Strategic Bioresource for a Sustainable Future. Bot. J. Linn. Soc. 2011, 166, 282–300. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  9. Tang, X.; Yuan, Y.; Wang, L.; Chen, S.; Liu, X.; Zhang, J. Identifying Prioritized Planting Areas for Medicinal Plant Thesium chinense Turcz. under Climate Change in China. Ecol. Inform. 2021, 66, 101459. [Google Scholar] [CrossRef] [Scilit]
  10. Wang, H.; Kang, C.; Zhang, W.; Zhou, L.; Wan, X.; Lyu, C.; Huang, L.; Liu, D.; Guo, L. Land Use Strategy of Ecological Agriculture of Chinese Materiamedica in Future Development. China J. Chin. Mater. Medica 2020, 45, 1990–1995. [Google Scholar] [CrossRef] [PubMed]
  11. Wang, W.; Xu, J.; Fang, H.; Li, Z.; Li, M. Advances and Challenges in Medicinal Plant Breeding. Plant Sci. 2020, 298, 110573. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  12. Chen, S.; Wei, J.; Huang, L.; Guo, B.; Xiao, P. Probing into the Theory Andpr Actice of Wild Medicinal Materials Tending. China J. Chin. Mater. Medica 2004, 29, 1123–1126. [Google Scholar]
  13. Trew, B.T.; Maclean, I.M.D. Vulnerability of Global Biodiversity Hotspots to Climate Change. Glob. Ecol. Biogeogr. 2021, 30, 768–783. [Google Scholar] [CrossRef] [Scilit]
  14. Parmesan, C.; Hanley, M.E. Plants and Climate Change: Complexities and Surprises. Ann. Bot. 2015, 116, 849–864. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  15. Trenberth, K.E. Climate Change Caused by Human Activities Is Happening and It Already Has Major Consequences. J. Energy Nat. Resour. Law 2018, 36, 463–481. [Google Scholar] [CrossRef] [Scilit]
  16. Sala, O.E.; Stuart Chapin, F., III; Armesto, J.J.; Berlow, E.; Bloomfield, J.; Dirzo, R.; Huber-Sanwald, E.; Huenneke, L.F.; Jackson, R.B.; Kinzig, A.; et al. Global Biodiversity Scenarios for the Year 2100. Science 2000, 287, 1770–1774. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  17. Kelly, A.E.; Goulden, M.L. Rapid Shifts in Plant Distribution with Recent Climate Change. Proc. Natl. Acad. Sci. USA 2008, 105, 11823–11826. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  18. Oliver, T.H.; Morecroft, M.D. Interactions between Climate Change and Land Use Change on Biodiversity: Attribution Problems, Risks, and Opportunities. WIREs Clim. Change 2014, 5, 317–335. [Google Scholar] [CrossRef] [Scilit]
  19. Donald, P.F.; Green, R.E.; Heath, M.F. Agricultural Intensification and the Collapse of Europe’s Farmland Bird Populations. Proc. R. Soc. Lond. B 2001, 268, 25–29. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  20. Benton, T.G.; Bryant, D.M.; Cole, L.; Crick, H.Q.P. Linking Agricultural Practice to Insect and Bird Populations: A Historical Study over Three Decades. J. Appl. Ecol. 2002, 39, 673–687. [Google Scholar] [CrossRef] [Scilit]
  21. Editorial Committee of Flora of China; Chinese Academy of Sciences. Flora Reipublicae Popularis Sinicae; Science Publishing Company: Beijing, China, 1996; Volume 30. [Google Scholar]
  22. National Pharmacopoeia Commission. Pharmacopoeia of the People’s Republic of China; China Medical Science Press: Beijing, China, 2020; Volume 1. [Google Scholar]
  23. Wang, Y.; Zhao, M.; Yu, J. A Study on the Dormancy Characteristic and Inner Inhibitory Substances of Fructus Schisandrae. China J. Chin. Mater. Medica 1997, 22, 10–12. [Google Scholar]
  24. Sun, B.; Lu, W.; Xu, P. Research Rrogress on the Reproductive and Cultivation Physilogyents and Main Active Ingredients of Schisandra chinensis. Heilongjiang Agric. Sci. 2023, 11, 10–18. [Google Scholar] [CrossRef]
  25. Pei, X. Establishment of Quality Evaluation System and Quality Standard for Seeds and Medicinal Materials of Schisandra chinensis. Master’s Thesis, Northwest A&F University, Yangling, China, 2025. [Google Scholar]
  26. Hu, L.; Zhang, H.; Qin, L.; Yan, B. Current Distribution of Schisandra chinensis in China and Its Predicted Responses to Climate Change. Chin. J. Appl. Ecol. 2012, 23, 2445–2450. [Google Scholar] [CrossRef]
  27. Lee, S.A.; Lee, S.; Ji, S.; Choi, J. Predicting Change of Suitable Plantation of Schisandra chinensis with Ensemble of Climate Change Scenario. Environ. Impact Assess. Rev. 2016, 25, 77–87. [Google Scholar] [CrossRef] [Scilit][Green Version]
  28. Mao, Y.; Wei, H.; Shang, Z.; Zhu, L.; Sang, M.; Gu, W. Habitat Suitability Assessment of Habitat Suitability Assessment of Schisandra chinensis (Turcz.) Baill. in Northeast China Based on GIS and Fuzzy Matter Element Model. Chin. J. Appl. Environ. Biol. 2016, 22, 241–248. [Google Scholar] [CrossRef] [Scilit]
  29. Zhang, D.; Xue, M.; Liu, M.; Shang, X.; Zhang, X.; Liu, J. Prediction of Potential Distribution of Schisandra chinensis and Schisandra sphenanthera Based on MaxEnt Model and Analysis of Its Important Influencing Factors. Hubei Agric. Sci. 2024, 63, 116–121. [Google Scholar] [CrossRef]
  30. Wang, D.; Li, C.; Zhu, C.; Li, X. Study on the Changes in Suitable Distribution Areas of Schisandra chinensis under Different Climate Change Patterns. Chin. Wild Plant Resour. 2025, 44, 92–99. [Google Scholar] [CrossRef]
  31. Stern, P.C.; Dietz, T. IPCC: Social Scientists Are Ready. Correspondence 2015, 521, 161. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  32. Gardner, A.S.; Maclean, I.M.D.; Gaston, K.J. Climatic Predictors of Species Distributions Neglect Biophysiologically Meaningful Variables. Divers. Distrib. 2019, 25, 1318–1333. [Google Scholar] [CrossRef] [Scilit]
  33. Li, Z.; He, X.; Liu, F.; Wang, J.; Feng, J. A Review of Polysaccharides from Schisandra chinensis and Schisandra sphenanthera: Properties, Functions and Applications. Carbohydr. Polym. 2018, 184, 178–190. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  34. Hao, R. Effects of Environmental Factors on Growth and Secondary Metabolism of Schisandra chinensis. Master’s Thesis, Northwest A&F University, Yangling, China, 2024. [Google Scholar]
  35. Xu, D.; Zhuo, Z.; Wang, R.; Ye, M.; Pu, B. Modeling the Distribution of Zanthoxylum armatum in China with MaxEnt Modeling. Glob. Ecol. Conserv. 2019, 19, e00691. [Google Scholar] [CrossRef] [Scilit]
  36. Warren, D.L.; Glor, R.E.; Turelli, M. ENMTools: A Toolbox for Comparative Studies of Environmental Niche Models. Ecography 2010, 33, 607–611. [Google Scholar] [CrossRef] [Scilit]
  37. Molaeinasab, A.; Bashari, H.; Esfahani, M.T.; Pourmanafi, S.; Toomanian, N.; Aghasi, B.; Jalalian, A. Predicting Soil Chemical Characteristics in the Arid Region of Central Iran Using Remote Sensing and Machine Learning Models. Sci. Rep. 2025, 15, 22809. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  38. Moya-Moraga, M.; Pérez-Ruíz, C. Application of MaxEnt Modeling and HRM Analysis to Support the Conservation and Domestication of Gevuina avellana Mol. in Central Chile. Plants 2022, 11, 2803. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  39. De Oliveira, T.M.L.; Lucas, F.M.F.; Camurugi, F.; Vieira, F.D.A. Could Bowdichia virgilicoides Be an Important Ally for Forest Restoration Under Climate Change Scenarios? Austral Ecol. 2026, 51, e70268. [Google Scholar] [CrossRef] [Scilit]
  40. Song, Y.; Xu, X.; Zhang, S.; Chi, X. Uncertainty Assessment of Species Distribution Prediction Using Multiple Global Climate Models on the Tibetan Plateau: A Case Study of Gentiana yunnanensis and Gentiana siphonantha. Land 2024, 13, 1376. [Google Scholar] [CrossRef] [Scilit]
  41. Hao, T.; Elith, J.; Guillera-Arroita, G.; Lahoz-Monfort, J.J. A Review of Evidence about Use and Performance of Species Distribution Modelling Ensembles like BIOMOD. Divers. Distrib. 2019, 25, 839–852. [Google Scholar] [CrossRef] [Scilit]
  42. Uusitalo, R.; Siljander, M.; Culverwell, C.L.; Mutai, N.C.; Forbes, K.M.; Vapalahti, O.; Pellikka, P.K.E. Predictive Mapping of Mosquito Distribution Based on Environmental and Anthropogenic Factors in Taita Hills, Kenya. Int. J. Appl. Earth Obs. Geoinf. 2019, 76, 84–92. [Google Scholar] [CrossRef] [Scilit]
  43. Thuiller, W. Ecological Niche Modelling. Curr. Biol. 2024, 34, R225–R229. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  44. Morales, N.S.; Fernández, I.C.; Baca-González, V. MaxEnt’s Parameter Configuration and Small Samples: Are We Paying Attention to Recommendations? A Systematic Review. PeerJ 2017, 5, e3093. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  45. Cobos, M.E.; Peterson, A.T.; Barve, N.; Osorio-Olvera, L. Kuenm: An R Package for Detailed Development of Ecological Niche Models Using Maxent. PeerJ 2019, 7, e6281. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  46. Barbet-Massin, M.; Jiguet, F.; Albert, C.H.; Thuiller, W. Selecting Pseudo-absences for Species Distribution Models: How, Where and How Many? Methods Ecol. Evol. 2012, 3, 327–338. [Google Scholar] [CrossRef] [Scilit]
  47. Liu, C.; Newell, G.; White, M. The Effect of Sample Size on the Accuracy of Species Distribution Models: Considering Both Presences and Pseudo-absences or Background Sites. Ecography 2019, 42, 535–548. [Google Scholar] [CrossRef] [Scilit]
  48. Mouton, A.M.; De Baets, B.; Goethals, P.L.M. Ecological Relevance of Performance Criteria for Species Distribution Models. Ecol. Model. 2010, 221, 1995–2002. [Google Scholar] [CrossRef] [Scilit]
  49. Zhao, G.; Cui, X.; Sun, J.; Li, T.; Wang, Q.; Ye, X.; Fan, B. Analysis of the Distribution Pattern of Chinese Ziziphus jujuba under Climate Change Based on Optimized Biomod2 and MaxEnt Models. Ecol. Indic. 2021, 132, 108256. [Google Scholar] [CrossRef] [Scilit]
  50. Hu, C.; Wu, H.; Zhang, G. Evaluating Habitat Suitability for the Endangered Sinojackia xylocarpa (Styracaceae) in China Under Climate Change Based on Ensemble Modeling and Gap Analysis. Biology 2025, 14, 304. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  51. Allouche, O.; Tsoar, A.; Kadmon, R. Assessing the Accuracy of Species Distribution Models: Prevalence, Kappa and the True Skill Statistic (TSS). J. Appl. Ecol. 2006, 43, 1223–1232. [Google Scholar] [CrossRef] [Scilit]
  52. Zhang, N.; Yu, K.; Wei, F.; Ma, S. On the Quality Essence and Evaluation Method of Traditional Chinese Medicinal Materials. Chin. Pharm. Aff. 2018, 32, 48–53. [Google Scholar] [CrossRef]
  53. Camacho, J.; Picó, J.; Ferrer, A. Data Understanding with PCA: Structural and Variance Information Plots. Chemom. Intell. Lab. Syst. 2010, 100, 48–56. [Google Scholar] [CrossRef] [Scilit]
  54. Peng, C.; Chen, L.; Zhang, G.; Sun, J. A Machine-Learning Model for Identifying Characteristics and Driving Factors of Lake Ice Phenology Changes in Northeast China. J. Lake Sci. 2026, 38, 1281–1294. [Google Scholar] [CrossRef] [Scilit]
  55. Kruk, M. SHAP-NET, a Network Based on Shapley Values as a New Tool to Improve the Explainability of the XGBoost-SHAP Model for the Problem of Water Quality. Environ. Model. Softw. 2025, 188, 106403. [Google Scholar] [CrossRef] [Scilit]
  56. Jiang, P.; Qin, M.; Li, R.; Meng, Y.; Yang, F.; Wen, R.; Sun, P.; Fang, Y. Seasonal Variability of GPP and Its Influencing Factors in the Typical Ecosystems in China. Ecol. Environ. Sci. 2022, 31, 643–651. [Google Scholar] [CrossRef]
  57. Tranmer, M.; Murphy, J.; Elliot, M.; Pampaka, M. Multiple Linear Regression, 2nd ed.; The University of Manchester: Manchester, UK, 2020. [Google Scholar]
  58. Moilanen, A. Landscape Zonation, Benefit Functions and Target-Based Planning: Unifying Reserve Selection Strategies. Biol. Conserv. 2007, 134, 571–579. [Google Scholar] [CrossRef] [Scilit]
  59. Yang, L.; Yang, L.; Li, J.; Zhang, C.; Huo, Z.; Luan, X. Potential Distribution and Conservation Priority Areas of Five Species in Northeast China. Acta Ecol. Sin. 2019, 39, 1082–1094. [Google Scholar] [CrossRef] [Scilit]
  60. Moilanen, A.; Franco, A.M.A.; Early, R.I.; Fox, R.; Wintle, B.; Thomas, C.D. Prioritizing Multiple-Use Landscapes for Conservation: Methods for Large Multi-Species Planning Problems. Proc. R. Soc. B. 2005, 272, 1885–1891. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  61. Liu, M.; Xie, X.; Liu, H.; Tian, W.; Wen, C.; Xin, Q. Study on Artificial Tending Techniques of Wild Forsythia Suspense in Taihang Mountain Area of Hebei Province. Lishizhen Med. Mater. Medica Res. 2008, 19, 2821–2822. [Google Scholar]
  62. Zhang, X.; Guo, L.; Zhou, T.; Huang, L. Discussion on Theory and Indes System of Ch Inesem Aterialm Ed Ical Regionalization. China J. Chin. Mater. Medica 2010, 35, 2350–2354. [Google Scholar]
  63. Li, N.; Xu, G. Grid Analysis of Land Use Based on Natural Breaks (Jenks) Classification. Bull. Surv. Mapp. 2020, 4, 106–110. [Google Scholar] [CrossRef]
  64. Yang, L.; Chen, M.; Challender, D.W.S.; Waterman, C.; Zhang, C.; Huo, Z.; Liu, H.; Luan, X. Historical Data for Conservation: Reconstructing Range Changes of Chinese Pangolin (Manis Pentadactyla) in Eastern China (1970–2016). Proc. R. Soc. B. 2018, 285, 20181084. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  65. Feng, K.; Wang, S.; He, Q.; Bonkowski, M.; Bahram, M.; Yergeau, E.; Wang, Z.; Peng, X.; Wang, D.; Li, S.; et al. CoBacFM: Core Bacteria Forecast Model for Global Grassland pH Dynamics under Future Climate Warming Scenarios. One Earth 2024, 7, 1275–1287. [Google Scholar] [CrossRef] [Scilit]
  66. Qiao, H. Thoughts on the Application of Species Distribution Models in Macroecology and Biogeography. Biodivers. Sci. 2026, 34, 25238. [Google Scholar] [CrossRef] [Scilit]
  67. Barbosa, W.L.; Alves-Souza, S.N. Data Quality Issues in Data Used in Species Distribution Models: A Systematic Literature Review. Ecol. Inform. 2025, 91, 103378. [Google Scholar] [CrossRef] [Scilit]
  68. Petrozzi, F.; Luiselli, L. When Big Data Misleads: Limitations of Large-Scale Online Biodiversity Databases for Species Distribution Modelling. J. Trop. Ecol. 2026, 42, e24. [Google Scholar] [CrossRef] [Scilit]
  69. Sun, Y.; Xiang, D.; Wang, J.; Jiang, K.; Zhu, H.; Huang, S.; Zhang, F.; Li, Y.; Zhang, H. Comparative Analysis of Modeling Methods and Prediction Accuracy for Japanese Sardine Habitat under Three Climate Scenarios with Differing Greenhouse Emission Pathways. Mar. Pollut. Bull. 2025, 215, 117867. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  70. Zhao, Y.; Liu, J.; Wang, Q.; Huang, R.; Nie, W.; Yang, S.; Cheng, X.; Li, M. Occurrence Data Sources Matter for Species Distribution Modeling: A Case Study of Quercus variabilis Based on Biomod2. Ecol. Evol. 2025, 15, e71390. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  71. Anselmetto, N.; Morresi, D.; Barbarino, S.; Loglisci, N.; Betts, M.G.; Garbarino, M. Species Distribution Models Built with Local Species Data Perform Better for Current Time, but Suffer from Niche Truncation. Agric. For. Meteorol. 2025, 362, 110361. [Google Scholar] [CrossRef] [Scilit]
  72. Soley-Guardia, M.; Alvarado-Serrano, D.F.; Anderson, R.P. Top Ten Hazards to Avoid When Modeling Species Distributions: A Didactic Guide of Assumptions, Problems, and Recommendations. Ecography 2024, 2024, e06852. [Google Scholar] [CrossRef] [Scilit]
  73. Nakamura, Y.; Krestov, P.V.; Omelko, A.M. Bioclimate and Zonal Vegetation in Northeast Asia: First Approximation to an Integrated Study. Phytocoenologia 2007, 37, 443–470. [Google Scholar] [CrossRef] [Scilit]
  74. Liu, Y.; Wang, X.; Guo, M.; Tani, H.; Matsuoka, N.; Matsumura, S. Spatial and Temporal Relationships among NDVI, Climate Factors, and Land Cover Changes in Northeast Asia from 1982 to 2009. GISci. Remote Sens. 2011, 48, 371–393. [Google Scholar] [CrossRef] [Scilit]
  75. Altmanová, N.; Fibich, P.; Doležal, J.; Bažant, V.; Černý, T.; Molina, J.G.A.; Enoki, T.; Hara, T.; Hoshizaki, K.; Ida, H.; et al. Spatial Heterogeneity of Tree-Growth Responses to Climate across Temperate Forests in Northeast Asia. Agric. For. Meteorol. 2025, 362, 110355. [Google Scholar] [CrossRef] [Scilit]
  76. Guenni, L.; Rose, C.W.; Hogarth, W.; Braddock, R.D.; Charles-Edwards, D. Seasonal Changes in Interrelationships between Climatic Variables. Agric. For. Meteorol. 1990, 53, 45–58. [Google Scholar] [CrossRef] [Scilit]
  77. Li, B. Resource Survey and Quality Evaluation of Schisandra chinensis. Master’s Thesis, Liaoning University of Traditional Chinese Medicine, Shenyang, China, 2008. [Google Scholar]
  78. Ding, Y.; Li, Z.; Peng, S. Global Analysis of Time-Lag and -Accumulation Effects of Climate on Vegetation Growth. Int. J. Appl. Earth Obs. Geoinf. 2020, 92, 102179. [Google Scholar] [CrossRef] [Scilit]
  79. Zhong, Z. Theories and Research Methods on the Behavioural Ecology of Climbing Plants; Science Press: Beijing, China, 2005. [Google Scholar]
  80. Wang, Y.; Wei, X. Advance on the Effects of Different Light Environments on Growth Physiological Biochemnistry and Morphostructure of Plant. J. Mt. Agric. Biol. 2010, 29, 353–359. [Google Scholar] [CrossRef]
  81. Li, A.; Ai, J.; Wang, Y.; Sun, C. A Study on Inducing Differentiation of Female Flower in Schisandra chinensis (Turcz.) Baill. Spec. Wild Econ. Anim. Plant Res. 2002, 2, 12–15. [Google Scholar] [CrossRef]
  82. Liu, S.; Li, A.; Guo, C.; Liu, Y.; Guo, W.; Yao, Y. Phenological Observations on Schisandra chinensis and Impactof Meteorological Factors on Its Phenological Characteristics. J. Northeast. For. Unversity 2009, 37, 39–42. [Google Scholar] [CrossRef]
  83. Vitasse, Y.; Lenz, A.; Körner, C. The Interaction between Freezing Tolerance and Phenology in Temperate Deciduous Trees. Front. Plant Sci. 2014, 5, 541. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  84. Wang, X.; Chen, X.; Xu, J.; Ji, Y.; Du, X.; Gao, J. Precipitation Dominates the Allocation Strategy of Above- and Belowground Biomass in Plants on Macro Scales. Plants 2023, 12, 2843. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  85. Wang, Y. Functional Traits of Leaves and Fine Roots of Three Temperate Lianas Species. Master’s Thesis, Northeast Forestry University, Harbin, China, 2020. [Google Scholar]
  86. Reich, P.B.; Luo, Y.; Bradford, J.B.; Poorter, H.; Perry, C.H.; Oleksyn, J. Temperature Drives Global Patterns in Forest Biomass Distribution in Leaves, Stems, and Roots. Proc. Natl. Acad. Sci. USA 2014, 111, 13721–13726. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  87. Tang, H.; Song, X.; Jin, L.; Zhang, W.; Zheng, J.; Zhang, L.; Yu, Q.; Shi, Y.; Guan, X.; Zhang, Z.; et al. Root-Zone Temperature Drives Coordinated Photosynthesis, Root Architecture, and Metabolism Responses in Schisandra chinensis (Trucz.) Baill. Plants 2025, 14, 2595. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  88. Ding, Y.; Leppälammi-Kujansuu, J.; Helmisaari, H.-S. Fine Root Longevity and Below- and Aboveground Litter Production in a Boreal Betula pendula Forest. For. Ecol. Manag. 2019, 431, 17–25. [Google Scholar] [CrossRef] [Scilit]
  89. Davies, W.J. Responses of Plant Growth and Functioning to Changes in Water Supply in a Changing Climate. In Plant Growth and Climate Change; Morison, J.I.L., Morecroft, M.D., Eds.; Wiley: Hoboken, NJ, USA, 2006; pp. 96–117. [Google Scholar]
  90. Zhao, X.-N.; Huang, S.-J.; Zhao, J.-M.; Zhang, Y.-W. Gender Variation in a Monoecious Woody Vine Schisandra chinensis (Schisandraceae) in Northeast China. Ann. Bot. Fenn. 2013, 50, 209–219. [Google Scholar] [CrossRef] [Scilit]
  91. Zhao, S. The Phenomenon of Flower and Fruit Abscission in Schisandra chinensis. Rural Pract. Sci. Technol. Inf. 2008, 7, 30. [Google Scholar]
  92. Seo, Y.; Kim, B.; Lee, J.; Kim, J.; Park, K.; Park, C.; Ahn, Y.; Cha, S. Effects of Soil Water Potential and Nitrogen Fertilization on Characteristics of Photosynthesis and Chlorophyll Fluorescence Induction in Schisandra chinensis Baillon. Korean J. Soil Sci. Fertil. 2015, 48, 705–711. [Google Scholar] [CrossRef] [Scilit]
  93. IPCC. Climate Change 2023: Synthesis Report. Contribution of Working Groups I, II and III to the Sixth Assessment Report of the Intergovernmental Panel on Climate Change; IPCC: Geneva, Switzerland, 2023. [Google Scholar]
  94. Sun, Z.; Zhao, J.; Zhang, H.; Wang, Y.; Fan, L.; Zhang, Z.; Guo, X.; Ren, Z.; Xiong, T.; Du, W.; et al. Predicting the Start of the Growing Season in Boreal Forest Under High and Low Emission Scenarios. Earth’s Future 2025, 13, e2024EF005622. [Google Scholar] [CrossRef] [Scilit]
  95. Liu, T.; Si, Z.; Liu, Y. Based on the Prediction of Future Drought Evolution in Heilongjiang Province under the CMIP6 Model. Pearl River 2025, 46, 21–28. [Google Scholar] [CrossRef]
  96. Song, F.; Fan, X.; Song, R. Review of Mixed Forest Litter Decomposition Researches. Acta Ecol. Sin. 2010, 30, 221–225. [Google Scholar] [CrossRef] [Scilit]
  97. Chen, L.; Dai, C.; Yu, C.; Wang, R. Spatial and Temporal Variation Characteristics of Precipitation During 1980-2020 in Heilongjiang Province. Water Resour. Power 2023, 41, 5–8. [Google Scholar] [CrossRef]
  98. Faleiro, F.V.; Machado, R.B.; Loyola, R.D. Defining Spatial Conservation Priorities in the Face of Land-Use and Climate Change. Biol. Conserv. 2013, 158, 248–257. [Google Scholar] [CrossRef] [Scilit]
  99. Zhang, B.; Chen, B.; Zhou, X.; Zou, H.; Duan, D.; Zhang, X.; Zhang, X. Distribution and Protection of Thesium chinense Turcz. under Climate and Land Use Change. Sci. Rep. 2024, 14, 6475. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  100. Putz, F.E. The Natural History of Lianas on Barro Colorado Island, Panama. Ecology 1984, 65, 1713–1724. [Google Scholar] [CrossRef] [Scilit]
  101. Reinmann, A.B.; Hutyra, L.R. Edge Effects Enhance Carbon Uptake and Its Vulnerability to Climate Change in Temperate Broadleaf Forests. Proc. Natl. Acad. Sci. USA 2017, 114, 107–112. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  102. Chen, C.-Y.; Liu, S.-Y.; Yan, Y.; Yin, L.; Di, P.; Liu, H.-M.; Liu, H.-Z. Candidate Genes Involved in the Biosynthesis of Lignan in Schisandra chinensis Fruit Based on Transcriptome and Metabolomes Analysis. Chin. J. Nat. Med. 2020, 18, 684–695. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  103. Guo, H.; Wang, J.; Gao, H.; Meng, X. High-Temperature Condition Increases Lignanoid Biosynthesis of Schisandra chinensis Seeds via Reactive Oxygen Species. Pharmacogn. Res. 2019, 11, 72–77. [Google Scholar] [CrossRef] [Scilit]
  104. Gupta, A.; Rico-Medina, A.; Caño-Delgado, A.I. The Physiology of Plant Responses to Drought. Science 2020, 368, 266–269. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  105. Rao, M.J.; Zheng, B. The Role of Polyphenols in Abiotic Stress Tolerance and Their Antioxidant Properties to Scavenge Reactive Oxygen Species and Free Radicals. Antioxidants 2025, 14, 74. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  106. Ninkuu, V.; Aluko, O.O.; Yan, J.; Zeng, H.; Liu, G.; Zhao, J.; Li, H.; Chen, S.; Dakora, F.D. Phenylpropanoids Metabolism: Recent Insight into Stress Tolerance and Plant Development Cues. Front. Plant Sci. 2025, 16, 1–21. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  107. Ri, I.; Pak, S.; Pak, U.; Yun, C.; Tang, Z. How Does UV-B Radiation Influence the Photosynthesis and Secondary Metabolism of Schisandra chinensis Leaves? Ind. Crops Prod. 2024, 208, 117832. [Google Scholar] [CrossRef] [Scilit]
  108. Singh, P.; Arif, Y.; Bajguz, A.; Hayat, S. The Role of Quercetin in Plants. Plant Physiol. Biochem. 2021, 166, 10–19. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  109. Xu, Q.; Guo, L.; Liu, Y.; Gao, Y. Effects of Potassium and Silicon Fertilization on Lignin Metabolism and Lodging Resistance of Oil Flax Stem. Chin. J. Eco-Agric. 2022, 30, 1451–1462. [Google Scholar] [CrossRef]
  110. Adam, M.; Ibrahim, I.; Sulieman, M.; Zeraatpisheh, M.; Mishra, G.; Brevik, E.C. Predicting Soil Cation Exchange Capacity in Entisols with Divergent Textural Classes: The Case of Northern Sudan Soils. Air Soil Water Res. 2021, 14, 1–14. [Google Scholar] [CrossRef] [Scilit]
  111. Amooh, M.K.; Bonsu, M. Effects of Soil Texture and Organic Matter on Evaporative Loss of Soil Moisture. J. Glob. Agric. Ecol. 2015, 3, 152–161. [Google Scholar]
  112. Whitmore, J.S. Vegetables for Drought-Prone Areas. In Drought Management on Farmland; Water Science and Technology Library; Springer: Dordrecht, The Netherlands, 2000; Volume 35, pp. 106–111. [Google Scholar]
  113. Shil, S.; Dewanjee, S. Impact of Drought Stress Signals on Growth and Secondary Metabolites (SMs) in Medicinal Plants. J. Phytopharm. 2022, 11, 371–376. [Google Scholar] [CrossRef] [Scilit]
  114. Al-Rawas, A.A.; Mohamedzein, Y.E.-A.; Al-Shabibi, A.S.; Al-Katheiri, S. Sand–Attapulgite Clay Mixtures as a Landfill Liner. Geotech. Geol. Eng. 2006, 24, 1365–1383. [Google Scholar] [CrossRef] [Scilit]
  115. Hei, J.; Li, Y.; Wang, Q.; Wang, S.; He, X. Effects of Exogenous Organic Acids on the Soil Metabolites and Microbial Communities of Panax Notoginseng from the Forest Understory. Agronomy 2024, 14, 601. [Google Scholar] [CrossRef] [Scilit]
  116. Wang, Y.; Lu, W.; Li, J.; Yang, Y.; Fan, S.; Wang, Y.; Qin, H.; Shu, N.; Zhang, B.; Li, C.; et al. Rhizosphere Microbiota and Soil Nutrients Shape Fruit Lignan Composition of Schisandra chinensis Across Temperate Cultivation Sites in Northeast and Northwest China. Life 2025, 15, 1555. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  117. Hu, H.; Bao, W.; Zhang, Q.; Li, F. Effect of Rock Fragment Content on Roots and Plant Growth: A Review. Chin. J. Appl. Environ. Biol. 2021, 27, 303–308. [Google Scholar] [CrossRef]
  118. Hu, H.; Bao, W.; Huang, L.; Li, F. Shifting Patterns in Fine Root Distribution of Four Xerophytic Species across Soil Structural Gradients and Years of Growth. Ecol. Evol. 2024, 14, e10889. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  119. Suresh, K.; Bhattacharyya, S.; Carvajal, J.; Ghosh, R.; Zeisler-Diehl, V.V.; Böckem, V.; Nagel, K.A.; Wojciechowski, T.; Schreiber, L. Effects of Water Stress on Apoplastic Barrier Formation in Soil Grown Roots Differ from Hydroponically Grown Roots: Histochemical, Biochemical and Molecular Evidence. Plant Cell Environ. 2024, 47, 4917–4931. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  120. Long, R.W.; Dudley, T.L.; D’Antonio, C.M.; Grady, K.C.; Bush, S.E.; Hultine, K.R. Spenders versus Savers: Climate-induced Carbon Allocation Trade-offs in a Recently Introduced Woody Plant. Funct. Ecol. 2021, 35, 1640–1654. [Google Scholar] [CrossRef] [Scilit]
  121. Jump, A.S.; Peñuelas, J. Running to Stand Still: Adaptation and the Response of Plants to Rapid Climate Change. Ecol. Lett. 2005, 8, 1010–1020. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  122. Cai, Y.; Zhu, P.; Liu, X.; Zhou, Y. Forest Fragmentation Trends and Modes in China: Implications for Conservation and Restoration. Int. J. Appl. Earth Obs. Geoinf. 2024, 133, 104094. [Google Scholar] [CrossRef] [Scilit]
  123. Zhang, L.; Zang, R. A Brief Analysis of the Cultivation of Schisandra chinensis. Spec. Econ. Anim. Plant 2007, 10, 36–37. [Google Scholar]
  124. Margules, C.R.; Pressey, R.L. Systematic Conservation Planning. Nature 2000, 405, 243–253. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  125. Harlio, A.; Kuussaari, M.; Heikkinen, R.K.; Arponen, A. Incorporating Landscape Heterogeneity into Multi-Objective Spatial Planning Improves Biodiversity Conservation of Semi-Natural Grasslands. J. Nat. Conserv. 2019, 49, 37–44. [Google Scholar] [CrossRef] [Scilit]
  126. Zhang, X. Study on the Quality Evaluation of Schisandra Chinensis Based on HPLC Characteristic Chromatogram and Multi-Test Evaluation. J. Chin. Med. Mater. 2024, 7, 1733–1737. [Google Scholar]
  127. Han, Z. Study on Quality Evaluation of Geo-authentic Traditional Chinese Drug in Liaoning Beiwuweizi (Schisandrae Chinensis Fructus) Based on Chemometrics and Fingerprint. Chin. Arch. Tradit. Chin. Med. 2024, 9, 69–73. [Google Scholar]
  128. Liu, Z. Establishment of Characteristic Pattern of Vinegar-processed Schisandra Chinensis Formula Granules and Content Determination of 5 Components. China Acad. J. Electron. Publ. 2021, 32, 1453–1459. [Google Scholar]
Figure 1. (a) Distribution point of S. chinensis; (b) Plant of S. chinensis; (c) Medicinal materials of S. chinensis (dried fruits).
Biology 15 01501 g001
Figure 2. (a) Distribution of the current suitable areas for S. chinensis across the entire ecological niche in Asia. (b) Proportion of current suitable areas in each country relative to the total suitable areas, where other countries include the Republic of Korea, Mongolia, Vietnam, Turkey and Georgia. (c) Proportion of current suitable areas in each province of China relative to the total current suitable areas of China, where other provinces include Hebei Province, Shanxi Province, Gansu Province, Chongqing Municipality, Guangxi Zhuang Autonomous Region, Hunan Province, Henan Province, Guangdong Province, Anhui Province, Jiangxi Province, Zhejiang Province and Fujian Province. (d) Distribution of current suitable areas for S. chinensis in Heilongjiang Province (1: The Greater Khingan Range; 2: Yilehuli Mountain; 3: The Lesser Khingan Range; 4: Zhangguangcai Range; 5: Laoye Range; 6: Wanda Mountain). (e) Area distribution of current low-, medium- and high-suitability areas for S. chinensis across all cities in Heilongjiang Province.
Biology 15 01501 g002
Figure 3. Changes in the distribution pattern of suitable growth areas of S. chinensis in Heilongjiang Province under the background of future global climate change.
Biology 15 01501 g003
Figure 4. Changes in the area of suitable areas for S. chinensis at each suitability level in Heilongjiang Province under future global climate change scenarios.
Biology 15 01501 g004
Figure 5. (a) The current land use situation within the suitable habitat area of S. chinensis in Heilongjiang Province. (b) The changes in the suitable habitat area of S. chinensis in Heilongjiang Province under the influence of global change. (c) Spatial pattern of suitable habitats for S. chinensis in Heilongjiang Province under global change.
Biology 15 01501 g005
Figure 6. Fingerprint patterns of 46 batches of S. chinensis and the control group(s) (The red dots indicate the apex positions of common peaks identified based on the reference spectrum.).
Biology 15 01501 g006
Figure 7. Distribution pattern of various chemical components of S. chinensis in Heilongjiang Province under current climate scenarios.
Biology 15 01501 g007
Figure 8. Changes in the areas of high-quality spatial distribution of various components of S. chinensis in Heilongjiang Province.
Biology 15 01501 g008
Figure 9. (a) The planning of three grades of protection areas for S. chinensis in Heilongjiang Province and their overlap with the current protected areas (the red numbers in (a) represent respectively: 1: Huzhong National Forest Park; 2: Fenghuangshan National Forest Park; 3: Heilongjiang Xiaobeihu Nature Reserve; 4: Danqinghe National Forest Park; and 5: Xiaoxing’anling National Geopark in Yichun City, Heilongjiang Province; 6: Muling Taxus cuspidata National Nature Reserve). (b) The overlapping area between the planned S. chinensis conservation reserves in Heilongjiang Province and existing conservation reserves, as well as the proportion of conservation reserves at all levels (the blue text in (b) indicates the overlapping area between the planned protected areas and the current protected areas).
Biology 15 01501 g009
Figure 10. (a) Hotspot counties for wild tending of S. chinensis with comprehensive active components in Heilongjiang Province under current climate scenarios. (b) Hotspot counties for wild tending of S. chinensis with high Schisandrol A content in Heilongjiang Province under current climate scenarios. (c) Hotspot counties for wild tending of S. chinensis with high Gomisin A content in Heilongjiang Province under current climate scenarios. (d) Hotspot counties for wild tending of S. chinensis with high Angeloylgomisin H content in Heilongjiang Province under current climate scenarios. (e) Hotspot counties for wild tending of S. chinensis with high Schizandrin B content in Heilongjiang Province under current climate scenarios. (f) Hotspot counties for wild tending of S. chinensis with high Schisantherin B content in Heilongjiang Province under current climate scenarios.
Biology 15 01501 g010
Table 1. VIF values of environmental factors.
FactorsVIFFactorsVIF
bio022.581t_caco31.658
bio082.538t_caso41.347
bio136.192t_clay1.805
bio144.774t_esp1.289
bio153.099t_gravel1.258
bio184.295t_oc1.190
bio194.843t_sand1.948
srad_summer2.843t_silt1.932
srad_winter3.672
Table 2. Optimal regression models for the contents of 6 chemical components.
Response VariableOptimal Linear ModelR2adjp-Value
ypcypc = 0.3364 × bio030.092980.02228 *
ySchisandrol AySchisandrol A = 0.3326 × bio02 + 0.7590 × t_cec_clay − 0.5768 × t_cec_soil + 0.3517 × t_ph_H2O0.150.02982 *
yGomisin AyGomisin A = 0.2690 × bio02 − 0.2949 × bio14 − 0.3111 × srad_summer0.20570.005298 **
yAngeloylgomisin HyAngeloylgomisin H = 0.4163 × bio02 − 0.3522 × srad_summer0.17550.005934 **
ySchizandrin BySchizandrin B = 0.3117 × bio03 − 0.2791 × t_gravel0.10540.03435 *
ySchisantherin BySchisantherin B = 0.3294 × t_ph_H2O0.088230.0254 *
*: p < 0.05; **: p < 0.01.
Table 3. Comparison of data sources, models, and climate scenarios used in the simulation study of S. chinensis potential suitable zones.
Serial NumberModeling AreaClimate ScenariosDistribution Data SourceModelSource
1ChinaCurrent and future 5 climate scenariosMainly derived from field surveys, online species distribution databases, and literature searchesMaxEnt[26]
2Republic of KoreaCurrent and future 5 climate scenariosPrimarily from field surveysMaxEnt[27]
3Northeastern China’s three provinces and northeastern Inner MongoliaCurrent climate scenarioPrimarily sourced from the Species Distribution Online Database and literature searchesFuzzy matter-element model[28]
4ChinaCurrent climate scenarioPrimarily sourced from the Species Distribution Online DatabaseMaxEnt[29]
5ChinaCurrent and future 10 climate scenariosPrimarily sourced from the Species Distribution Online DatabaseMaxEnt[30]
6Asia (full ecological niche)Current and future 17 climate scenariosPrimarily sourced from field surveys, online species distribution databases, literature searches, and the plantR packageBiomod2 modelThis Study
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.