

Pesticide Degradation by Soil Bacteria: Mechanisms, Bioremediation Strategies, and Implications for Sustainable Agriculture




Abstract
1. Introduction
2. Pesticide Classes and Environmental Persistence

| Pesticide Class | Representative Compounds | Average Soil Half-Life (DT50) | Persistence Category | Sources |
|---|---|---|---|---|
| Organophosphates | Chlorpyrifos, Parathion | 30–60 days | Moderate | [33,42] |
| Carbamates | Carbofuran, Aldicarb | 10–50 days | Low to Moderate | [23,43] |
| Pyrethroids | Cypermethrin, Permethrin | 30–100 days (up to years in anaerobic conditions) | Moderate to High | [40,44,45] |
| Neonicotinoids | Imidacloprid, Acetamiprid | 40–150 days (dry conditions longer) | Moderate | [31,41,46,47,48] |
| Triazines | Atrazine, Simazine | 60–100 days | Moderate | [49,50] |
| Organochlorines | DDT, Chlordane | 2–15 years | High | [3,11] |
| Others (e.g., Glyphosate) | Glyphosate | 3–5 days (variable) | Low | [30,51] |
3. Bacterial Taxa Involved in Pesticide Degradation
| Bacterial Genus/Species | Pesticides Degraded | Process/Notes | Sources |
|---|---|---|---|
| Pseudomonas | Organophosphates, Pyrethroids, DDT, Phenolics | Hydrolysis, Oxidation,/genetically modified for phenolics; consortia synergy and PTE/OPH-mediated cleavage of P–O bonds in organophosphates | [10,53,54,61] |
| Rhodococcus | Endosulfan, Triazines, Chlorpyrifos | Oxidation, ring cleavage/Produces metabolites such as endosulfan diol monosulfate in soil | [58,59,60,64] |
| Arthrobacter aurescens TC1 | Atrazine, S-Triazines | Hydrolytic dechlorination, ring-cleavage/Specialized pathways for s-triazine metabolism | [61,63,65] |
| Bacillus | Pyrethroids, Diphenyl Ethers, Carbamates | Ester hydrolysis, nitroreduction/Enhanced rates in consortia; some strains dissipate triazoles | [60,66,67,68,69] |
| Burkholderia | Parathion, Carbofuran, Various Organochlorines | Hydrolysis, oxidation/Broad-spectrum degradation; cometabolism supported by plant rhizosphere | [9,12,70,71] |
| Flavobacterium | Organophosphates | Hydrolysis/Early-identified OP-degrading genus | [9,10,12] |
| Klebsiella | Neonicotinoids, Chlorpyrifos | Ester hydrolysis/Nitroreductases assist detoxification | [72,73,74] |
| Novosphingobium | PAHs, Sulfonylureas, Neonicotinoids | Oxidation, hydrolysis/Dioxygenases contribute to aromatic ring cleavage | [75] |
| Acinetobacter | Neonicotinoids, Diazinon, Organophosphates | Hydrolysis/achieves up to 80% diazinon removal in laboratory systems and contributes to OP and neonicotinoid dissipation in contaminated soils | [72,73,76] |
| Streptomyces | DDT, Endosulfan, Diflufenican Carbamates, Organophosphates | Oxidation, cometabolism/actinobacterial degradation important in pesticide-enriched agricultural soils and biomixtures | [46,73,77] |
| Sphingomonas | Neonicotinoids, Sufonylureas | Oxidation, hydrolysis/genetically modified for carbamates/organophosphates; biofilm enhances stability and cytochrome P450 monooxygenases enable oxidative breakdown of neonicotinoids | [52,78] |
| Stenotrophomonas | Neonicotinoids, Sufonylureas | Hydrolysis, cometabolism/tolerates co-contaminants and contributes to sulfonylurea dissipation in multi-pesticide systems | [26,79] |
| Alcaligenes | Organochlorines | Reductive dichlorination/targets persistent organochlorine pollutants via stepwise removal of chlorine substituents | [80] |
| Achromobacter | Triazines | Hydrolysis, ring-cleavage/active in agricultural soils where it contributes to triazine herbicide dissipation | [44,81] |
| Paracoccus | Pyrethroids | Ester hydrolysis/catalyzes initial detoxification of pyrethroids, producing more polar intermediates for further microbial metabolism | [26,82] |
4. Enzymatic and Genetic Mechanisms of Degradation
5. Environmental Factors Affecting Degradation
| Environmental Factor | Effect on Degradation | Indicative Optimal Range | Notes/Interpretation | Example Pesticides/Bacteria Affected | Source |
|---|---|---|---|---|---|
| pH | Controls enzyme stability, hydrolysis rates, sorption interactions | Neutral (pH 6–7) | Acidic soils (<5.5) reduce pyrethroid degradation; OP hydrolysis faster near neutral | Chlorpyrifos/Pseudomonas (optimal pH 7); Atrazine/Arthrobacter (unaffected 5.5–8.5); Lindane/Bacillus (peak at pH 8) | [89,136,137,138,139,140,141,142,143] |
| Temperature | Increase enzyme kinetics and microbial metabolism | 25–30 °C | Degradation declines rapidly < (15 °C | Lindane/soil consortia (optimal 30 °C, 60% degradation); Chlorpyrifos/Rhodococcus (faster at 28 °C); General pesticides (slowed at 1.9–15 °C) | [141,144,145,146,147,148,149] |
| Moisture/Water holding | Support microbial growth and substrate diffusion, biomass and nutrient transfer | Field capacity (60–80%) | Drought and waterlogging inhibit microbial activity | Pyrethroids/Bacillus (50% WHC optimal); Neonicotinoids/Sphingomonas (reduced at low moisture/ <50% WHC) | [141,145,146,147,148,149] |
| Organic Matter (OM)/Organic compounds | Supports cometabolism + microbial adaptation; also increases sorption | 2–5% OM | Elevated OM increases sorption affinity (higher Koc) and reduces pesticide bioavailability; balanced OM improves co-metabolism | Atrazine/indigenous consortia (>3% SOM accelerates); Carbamates (compost amendments enhance 30–50%) | [89,141,150,151,152,153,154] |
| Aeration/Oxygen | Enable aerobic monooxygenases and oxidase reaction | Air-filled porosity ≥ 10–15% | Below ~10% AFP aerobic turnover drops; compaction & flooding limit O2 | DDT/soil bacteria (both conditions viable, aerobic faster); Clothianidin (rapid anaerobic at 25–35 °C); Aldicarb (faster anaerobic) | [136,155,156,157,158,159,160,161,162] |
6. Bioremediation Strategies
6.1. Natural Attenuation
6.2. Bioaugmentation
6.3. Synthetic Microbial Consortia
6.4. Field-Scale Applications
7. Methodology
8. Advances in Omics Technologies and Synthetic Biology
9. Regulatory and Practical Considerations
10. Implications for Sustainable Agriculture
11. Conclusions
Author Contributions
Funding
Data Availability Statement
Acknowledgments
Conflicts of Interest
Abbreviations
| 3,5,6-TCP | 3,5,6-Trichloro-2-pyridinol |
| AHL | Acyl-homoserine lactone |
| AMPA | Aminomethylphosphonic acid |
| BCF | Bioconcentration Factor |
| CFU | Colony Forming Unit |
| CP | Chlorpyrifos |
| DDT | Dichlorodiphenyltrichloroethane |
| DT50 | Dissipation Half-Life (time required for 50% degradation) |
| EBDC | Ethylene bis-dithiocarbamate |
| FC | Field Capacity |
| NH4+ | Ammonium |
| GMO | Genetically modified organism |
| OM | Organic Matter |
| OP | Organophosphate |
| OPH | Organophosphorus Hydrolase |
| PAH | Polycyclic Aromatic Hydrocarbon |
| PTE | Phosphotriesterase |
| QS | Quorum Sensing |
| RH | Relative Humidity |
| SOM | Soil Organic Matter |
| UV | Ultraviolet Radiation |
| WHC | Water Holding Capacity |
References
- Aktar, M.W.; Sengupta, D.; Chowdhury, A. Impact of pesticides use in agriculture: Their benefits and hazards. Interdiscip. Toxicol. 2009, 2, 1–12. [Google Scholar] [CrossRef] [Scilit]
- FAO. The State of Food and Agriculture 2023: Revealing the True Cost of Food to Transform Agrifood Systems. Food and Agriculture Organization of the United Nations. 2023. Available online: https://www.fao.org/documents/card/en/c/cc7724en (accessed on 21 August 2025).
- Bouwman, H.; Sereda, B.; Meinhardt, H.M. Simultaneous presence of DDT and pyrethroid residues in human breast milk from a malaria-endemic area in South Africa. Environ. Pollut. 2003, 156, 902–917. [Google Scholar] [CrossRef] [Scilit]
- Sharma, A.; Kumar, V.; Shahzad, B.; Tanveer, M.; Sidhu, G.; Handa, N.; Kohli, S.; Yadav, P.; Bali, A.; Parihar, R.; et al. Worldwide pesticide usage and its impacts on ecosystem. SN Appl. Sci. 2019, 1, 1446. [Google Scholar] [CrossRef] [Scilit]
- Kim, K.H.; Kabir, E.; Jahan, S.A. Exposure to pesticides and the associated human health effects. Sci. Total Environ. 2024, 904, 166147. [Google Scholar] [CrossRef] [Scilit]
- Nicolopoulou-Stamati, P.; Maipas, S.; Kotampasi, C.; Stamatis, P.; Hens, L. Chemical pesticides and human health: The urgent need for a new concept in agriculture. Front. Public Health 2016, 4, 148. [Google Scholar] [CrossRef] [Scilit]
- Chaudhary, V.; Kumar, M.; Chauhan, C.; Sirohi, U.; Srivastav, A.L.; Rani, L. Strategies for mitigation of pesticides from the environment through alternative approaches: A review of recent developments and future prospects. J. Environ. Manag. 2024, 354, 120326. [Google Scholar] [CrossRef] [Scilit]
- Mnif, W.; Hassine, A.I.H.; Bouaziz, A.; Bartegi, A.; Thomas, O.; Roig, B. Effect of endocrine disruptor pesticides: A review. Int. J. Environ. Res. Public Health 2011, 8, 2265–2303. [Google Scholar] [CrossRef] [Scilit]
- Bose, S.; Kumar, P.S.; Vo, D.V.N.; Rajamohan, N.; Saravanan, R. Microbial degradation of recalcitrant pesticides: A review. Environ. Chem. Lett. 2021, 19, 3209–3228. [Google Scholar] [CrossRef] [Scilit]
- Singh, B.K.; Walker, A. Microbial degradation of organophosphorus compounds. FEMS Microbiol. Rev. 2006, 30, 428–471. [Google Scholar] [CrossRef] [Scilit]
- Ortiz-Hernández, M.L.; Sánchez-Salinas, E.; Dantán-González, E.; Castrejón-Godínez, M.L. Pesticide biodegradation: Mechanisms, genetics and strategies to enhance the process. In BT-Biodegradation-Life of Science; Intechopen: London, UK, 2013; pp. 251–287. [Google Scholar] [CrossRef] [Scilit]
- Lopes, P.R.M.; Cruz, V.H.; de Menezes, A.B.; Gadanhoto, B.P.; Moreira, B.R.A.; Mendes, C.R.; Mazzeo, D.E.C.; Dilarri, G.; Montagnolli, R.N. Microbial bioremediation of pesticides in agricultural soils: An integrative review on natural attenuation, bioaugmentation and biostimulation. Rev. Environ. Sci. Biotechnol. 2022, 21, 851–876. [Google Scholar] [CrossRef] [Scilit]
- Morillo, E.; Villaverde, J. Advanced technologies for the remediation of pesticide-contaminated soils. Sci. Total Env. 2017, 586, 576–597. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sahoo, A.; Yadav, G.; Mehta, T.; Meena, M.; Swapnil, P. Omics-driven insights into plant growth-promoting microorganisms for sustainable agriculture. Discov. Sustain. 2025, 6, 659. [Google Scholar] [CrossRef] [Scilit]
- Rayu, S.; Nielsen, U.N.; Nazaries, L.; Singh, B.K. Isolation and molecular characterization of novel chlorpyrifos and 3,5,6-trichloro-2-pyridinol-degrading bacteria from sugarcane farm soils. Front. Microbiol. 2017, 8, 518. [Google Scholar] [CrossRef] [Scilit]
- Chennappa, G.; Udaykumar, N.; Vidya, M.; Nagaraja, H.; Amaresh, Y.S.; Sreenivasa, M.Y. Azotobacter—A Natural Resource for Bioremediation of Toxic Pesticides in Soil Ecosystems. In New and Future Developments in Microbial Biotechnology and Bioengineering; Elsevier: Amsterdam, The Netherlands, 2019; pp. 267–279. [Google Scholar] [CrossRef] [Scilit]
- Arbeli, Z.; Fuentes, C.L. Microbial Degradation of Pesticides in Tropical Soils. In Biodegradation of Pesticides; Springer: New York, NY, USA, 2010; pp. 251–274. [Google Scholar] [CrossRef] [Scilit]
- UNEP. Global Chemicals Outlook II: From Legacies to Innovative Solutions. United Nations Environment Programme. 2021. Available online: https://www.unep.org/resources/report/global-chemicals-outlook-ii-legacies-innovative-solutions (accessed on 20 March 2025).
- Rayu, S.; Nielsen, U.N.; Nazaries, L.; Singh, B.K. Isolation and characterization of novel microbes for bioremediation of pesticides. Environ. Chem. 2017, 14, 387–400. [Google Scholar] [CrossRef] [Scilit]
- Arias, L.A.; Garzón, A.; Ayarza, A.; Aux, S.; Bojacá, C.R. Environmental fate of pesticides in open field and greenhouse tomato production regions from Colombia. Environ. Adv. 2021, 3, 100031. [Google Scholar] [CrossRef] [Scilit]
- Bhatt, P.; Zhou, X.; Huang, Y.; Zhang, W.; Chen, S. Characterization of the role of esterases in the biodegradation of organophosphate, carbamate, and pyrethroid pesticides. J. Hazard. Mater. 2021, 411, 125026. [Google Scholar] [CrossRef] [Scilit]
- Fenner, K.; Canonica, S.; Wackett, L.P.; Elsner, M. Evaluating pesticide degradation in the environment: Blind spots and emerging opportunities. Science 2013, 341, 752–758. [Google Scholar] [CrossRef] [Scilit]
- Malhotra, H.; Kaur, S.; Phale, P.S. Conserved Metabolic and Evolutionary Themes in Microbial Degradation of Carbamate Pesticides. Front. Microbiol. 2021, 12, 648868. [Google Scholar] [CrossRef] [Scilit]
- Mdeni, N.L.; Adeniji, A.O.; Okoh, A.I.; Okoh, O.O. Analytical Evaluation of Carbamate and Organophosphate Pesticides in Human and Environmental Matrices: A Review. Molecules 2022, 27, 618. [Google Scholar] [CrossRef] [Scilit]
- Zhou, W.; Li, M.; Achal, V. A comprehensive review on environmental and human health impacts of chemical pesticide usage. Emerg. Contam. 2025, 11, 100410. [Google Scholar] [CrossRef] [Scilit]
- Lei, Q.; Zhong, J.; Chen, S.-F.; Wu, S.; Huang, Y.; Guo, P.; Mishra, S.; Bhatt, K.; Chen, S. Microbial degradation as a powerful weapon in the removal of sulfonylurea herbicides. Environ. Res. 2023, 235, 116570. [Google Scholar] [CrossRef] [Scilit]
- Fenet, H.; Beltran, E.; Gadji, B.; Cooper, J.F.; Coste, C.M. Fate of a phenylpyrazole in vegetation and soil under tropical field conditions. J. Agric. Food Chem. 2001, 49, 1293–1297. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Satapute, P.; Kaliwal, B. Biodegradation of propiconazole by newly isolated Burkholderia sp. strain BBK_9. 3 Biotech. 2016, 6, 110. [Google Scholar] [CrossRef] [Scilit]
- Bhandari, G.; Atreya, K.; Scheepers, P.T.J.; Geissen, V. Concentration and distribution of pesticide residues in soil: Non-dietary human health risk assessment. Chemosphere 2020, 253, 126594. [Google Scholar] [CrossRef] [Scilit]
- Borggaard, O.K.; Gimsing, A.L. Fate of glyphosate in soil and the possibility of leaching to ground and surface waters: A review. Pest. Manag. Sci. 2008, 64, 441–456. [Google Scholar] [CrossRef] [Scilit]
- Goulson, D. An overview of the environmental risks posed by neonicotinoid insecticides. J. Appl. Ecol. 2013, 50, 977–987. [Google Scholar] [CrossRef] [Scilit]
- Arya, R.; Kumar, R.; Mishra, N.K.; Sharma, A.K. Microbial Flora and Biodegradation of Pesticides: Trends, Scope, and Relevance. In Advances in Environmental Biotechnology; Springer: Singapore, 2017; pp. 243–263. [Google Scholar] [CrossRef] [Scilit]
- Kumar, S.; Kaushik, G.; Dar, M.A.; Nimesh, S.; López-Chuken, U.J.; Villarreal-Chiu, J.F. Microbial Degradation of Organophosphate Pesticides: A Review. Pedosphere 2018, 28, 190–208. [Google Scholar] [CrossRef] [Scilit]
- Jayaraj, R.; Megha, P.; Sreedev, P. Organochlorine pesticides, their toxic effects on living organisms and their fate in the environment. Interdiscip. Toxicol. 2016, 9, 90–100. [Google Scholar] [CrossRef] [Scilit]
- Tzanetou, E.N.; Karasali, H. A Comprehensive Review of Organochlorine Pesticide Monitoring in Agricultural Soils: The Silent Threat of a Conventional Agricultural Past. Agriculture 2022, 12, 728. [Google Scholar] [CrossRef] [Scilit]
- Kamalesh, T.; Kumar, P.S.; Rangasamy, G. An insights of organochlorine pesticides categories, properties, eco-toxicity and new developments in bioremediation process. Environ. Pollut. 2023, 333, 122114. [Google Scholar] [CrossRef] [Scilit]
- Faroon, O.; Harris, M.O. Toxicological Profile for DDT, DDE, and DDD. ATSDR’s Toxicol. Profiles 2002. Available online: https://www.atsdr.cdc.gov/toxprofiles/tp35.pdf (accessed on 20 March 2025).
- Rani, L.; Thapa, K.; Kanojia, N.; Sharma, N.; Singh, S.; Grewal, A.S.; Srivastav, A.L.; Kaushal, J. An extensive review on the consequences of chemical pesticides on human health and environment. J. Clean. Prod. 2021, 283, 124657. [Google Scholar] [CrossRef] [Scilit]
- Kumari, A.; Dash, M.; Singh, S.K.; Jagadesh, M.; Mathpal, B.; Mishra, P.K.; Pandey, S.K.; Verma, K.K. Soil Microbes: A Natural Solution for Mitigating the Impact of Climate Change. Environ. Monit. Assess. 2023, 195, 1436. [Google Scholar] [CrossRef] [Scilit]
- Amweg, E.L.; Weston, D.P.; Ureda, N.M. Use and toxicity of pyrethroid pesticides in the Central Valley, California, USA. Environ. Toxicol. Chem. 2005, 24, 966–972. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bonmatin, J.M.; Giorio, C.; Girolami, V.; Goulson, D.; Kreutzweiser, D.P.; Krupke, C.; Liess, M.; Long, E.; Marzaro, M.; Mitchell, E.A.D.; et al. Environmental fate and exposure; neonicotinoids and fipronil. Environ. Sci. Pollut. Res. 2015, 22, 35–67. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bhende, R.S.; Jhariya, U.; Srivastava, S.; Bombaywala, S.; Das, S.; Dafale, N.A. Environmental Distribution, Metabolic Fate, and Degradation Mechanism of Chlorpyrifos: Recent and Future Perspectives. Appl. Biochem. Biotechnol. 2022, 194, 2301–2335. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mishra, S.; Pang, S.; Zhang, W.; Lin, Z.; Bhatt, P.; Chen, S. Insights into the microbial degradation and biochemical mechanisms of carbamates. Chemosphere 2021, 279, 130500. [Google Scholar] [CrossRef] [Scilit]
- Cycon, M.; Piotrowska-Seget, Z. Pyrethroid-degrading microorganisms and their potential for the bioremediation of contaminated soils: A review. Front. Microbiol. 2016, 7, 218351. [Google Scholar] [CrossRef] [Scilit]
- Zhan, H.; Huang, Y.; Lin, Z.; Bhatt, P.; Chen, S. New insights into the microbial degradation and catalytic mechanism of synthetic pyrethroids. Environ. Res. 2020, 182, 109138. [Google Scholar] [CrossRef] [Scilit]
- Briceño, G.; Fuentes, M.S.; Saez, J.M.; Diez, M.C.; Benimeli, C.S. Streptomyces Genus as Biotechnological Tool for Pesticide Degradation in Polluted Systems. Crit. Rev. Environ. Sci. Technol. 2018, 48, 773–805. [Google Scholar] [CrossRef] [Scilit]
- Anandhi, G.; Iyapparaja, M. Systematic approaches to machine learning models for predicting pesticide toxicity. Heliyon 2024, 10, e28752. [Google Scholar] [CrossRef] [Scilit]
- Simon-Delso, N.; Amaral-Rogers, V.; Belzunces, L.P.; Bonmatin, J.M.; Chagnon, M.; Downs, C.; Furlan, L.; Gibbons, D.W.; Giorio, C.; Girolami, V.; et al. Systemic insecticides (neonicotinoids and fipronil): Trends, uses, mode of action and metabolites. Environ. Sci. Pollut. Res. 2015, 22, 5–34. [Google Scholar] [CrossRef] [Scilit]
- Arias-Estévez, M.; López-Periago, E.; Martínez-Carballo, E.; Simal-Gándara, J.; Mejuto, J.C.; García-Río, L. The mobility and degradation of pesticides in soils and the pollution of groundwater resources. Agric. Ecosyst. Environ. 2008, 123, 247–260. [Google Scholar] [CrossRef] [Scilit]
- Graymore, M.; Stagnitti, F.; Allinson, G. Impacts of atrazine in aquatic ecosystems. Environ. Int. 2001, 26, 483–495. [Google Scholar] [CrossRef] [Scilit]
- Duke, S.O.; Powles, S.B. Glyphosate: A once-in-a-century herbicide. Pest. Manag. Sci. 2008, 64, 319–325. [Google Scholar] [CrossRef] [Scilit]
- Chia, X.K.; Hadibarata, T.; Kristanti, R.A.; Jusoh, M.N.H.; Tan, I.S.; Foo, H.C.Y. The function of microbial enzymes in breaking down soil contaminated with pesticides: A review. Bioprocess. Biosyst. Eng. 2024, 47, 597–620. [Google Scholar] [CrossRef] [Scilit]
- Gong, T.; Liu, R.; Zuo, Z.; Che, Y.; Yu, H.; Song, C.; Yang, C. Metabolic Engineering of Pseudomonas putida KT2440 for Complete Mineralization of Methyl Parathion and γ-Hexachlorocyclohexane. ACS Synth. Biol. 2016, 5, 434–442. [Google Scholar] [CrossRef] [Scilit]
- Zuo, Z.; Gong, T.; Che, Y.; Liu, R.; Xu, P.; Jiang, H.; Qiao, C.; Song, C.; Yang, C. Engineering Pseudomonas putida KT2440 for simultaneous degradation of organophosphates and pyrethroids and its application in bioremediation of soil. Biodegradation 2015, 26, 223–233. [Google Scholar] [CrossRef] [Scilit]
- Akbar, S.; Sultan, S.; Kertesz, M. Determination of Cypermethrin Degradation Potential of Soil Bacteria Along with Plant Growth-Promoting Characteristics. Curr. Microbiol. 2015, 70, 75–84. [Google Scholar] [CrossRef] [Scilit]
- Garbisu, C.; Garaiyurrebaso, O.; Epelde, L.; Grohmann, E.; Alkorta, I. Plasmid-mediated bioaugmentation for the bioremediation of contaminated soils. Front. Microbiol. 2017, 8, 1966. [Google Scholar] [CrossRef] [Scilit]
- Castro-Gutiérrez, V.; Fuller, E.; Thomas, J.C.; Sinclair, C.J.; Johnson, S.; Helgason, T.; Moir, J.W.B. Genomic basis for pesticide degradation revealed by selection, isolation and characterisation of a library of metaldehyde-degrading strains from soil. Soil. Biol. Biochem. 2020, 142, 107702. [Google Scholar] [CrossRef] [Scilit]
- Ito, K.; Kawashima, F.; Takagi, K.; Kataoka, R.; Kotake, M.; Kiyota, H.; Yamazaki, K.; Sakakibara, F.; Okada, S. Isolation of endosulfan sulfate-degrading Rhodococcus koreensis strain S1-1 from endosulfan contaminated soil and identification of a novel metabolite, endosulfan diol monosulfate. Biochem. Biophys. Res. Commun. 2016, 473, 1094–1099. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Verma, K.; Agrawal, N.; Farooq, M.; Misra, R.B.; Hans, R.K. Endosulfan degradation by a Rhodococcus strain isolated from earthworm gut. Ecotoxicol. Environ. Saf. 2006, 64, 377–381. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Huang, Y.; Chen, S.-F.; Chen, W.-J.; Zhu, X.; Mishra, S.; Bhatt, P.; Chen, S. Efficient biodegradation of multiple pyrethroid pesticides by Rhodococcus pyridinivorans strain Y6 and its degradation mechanism. Chem. Eng. J. 2023, 469, 143863. [Google Scholar] [CrossRef] [Scilit]
- Strong, L.C.; Rosendahl, C.; Johnson, G.; Sadowsky, M.J.; Wackett, L. Arthrobacter aurescens TC1 metabolizes diverse s-triazine ring compounds. Appl. Environ. Microbiol. 2002, 68, 5973–5980. [Google Scholar] [CrossRef] [Scilit]
- Sajjaphan, K.; Shapir, N.; Wackett, L.P.; Palmer, M.; Blackmon, B.; Tomkins, J.; Sadowsky, M.J. Arthrobacter aurescens TC1 atrazine catabolism genes trzN, atzB, and atzC are linked on a 160-kilobase region and are functional in Escherichia coli. Appl. Environ. Microbiol. 2004, 70, 4402–4407. [Google Scholar] [CrossRef] [Scilit]
- Li, Q.; Li, Y.; Zhu, X.; Cai, B. Isolation and characterization of atrazine-degrading Arthrobacter sAD26 and use of this strain in bioremediation of contaminated soil. J. Environ. Sci. 2008, 20, 1226–1230. [Google Scholar] [CrossRef] [Scilit]
- Zhao, T.; Hu, K.; Li, J.; Zhu, Y.; Liu, A.; Yao, K.; Liu, S. Current insights into the microbial degradation for pyrethroids: Strain safety, biochemical pathway, and genetic engineering. Chemosphere 2021, 279, 130542. [Google Scholar] [CrossRef] [Scilit]
- Mandelbaum, R.T.; Allan, D.L.; Wackett, L. Isolation and characterization of a Pseudomonas that mineralizes the s-triazine herbicide atrazine. Appl. Environ. Microbiol. 1995, 61, 1451–1457. [Google Scholar] [CrossRef] [Scilit]
- Tian, Y.; Zhao, G.; Cheng, M.; Lu, L.; Zhang, H.; Huang, X. A nitroreductase DnrA catalyzes the biotransformation of several diphenyl ether herbicides in Bacillus sp. Za. Appl. Microbiol. Biotechnol. 2023, 107, 5269–5279. [Google Scholar] [CrossRef] [Scilit]
- Farhan, M.; Ahmad, M.; Kanwal, A.; Butt, Z.A.; Khan, Q.F.; Raza, S.A.; Qayyum, H.; Wahid, A. Biodegradation of chlorpyrifos using isolates from contaminated agricultural soil, its kinetic studies. Sci. Rep. 2021, 11, 1–14. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Xiao, Y.; Lu, Q.; Yi, X.; Zhong, G.; Liu, J. Synergistic Degradation of Pyrethroids by the Quorum Sensing-Regulated Carboxylesterase of Bacillus subtilis BSF01. Front. Bioeng. Biotechnol. 2020, 8, 889. [Google Scholar] [CrossRef] [Scilit]
- Salunkhe, V.P.; Sawant, I.S.; Banerjee, K.; Wadkar, P.N.; Sawant, S.D. Enhanced Dissipation of Triazole and Multiclass Pesticide Residues on Grapes after Foliar Application of Grapevine-Associated Bacillus Species. J. Agric. Food Chem. 2015, 63, 10736–10746. [Google Scholar] [CrossRef] [Scilit]
- Ahmad, S.; Ahmad, H.W.; Bhatt, P. Microbial adaptation and impact into the pesticide’s degradation. Arch. Microbiol. 2022, 204, 1–25. [Google Scholar] [CrossRef] [Scilit]
- Bilal, M.; Ashraf, S.S.; Iqbal, H.M.N. Laccase-Mediated Bioremediation of Dye-Based Hazardous Pollutants. In Methods for Bioremediation of Water and Wastewater Pollution; Ahamed, M.I., Lichtfouse, E., Asiri, A.M., Eds.; Springer: Cham, Switzerland, 2020. [Google Scholar] [CrossRef] [Scilit]
- Pandey, R.; Sharma, A.; Kumar, V. Neonicotinoid degradation by Klebsiella and Acinetobacter: Enzymatic mechanisms. Environ. Technol. Innov. 2023, 30, 103098. [Google Scholar] [CrossRef] [Scilit]
- Pang, S.; Lin, Z.; Zhang, W.; Mishra, S.; Bhatt, P.; Chen, S. Insights Into the Microbial Degradation and Biochemical Mechanisms of Neonicotinoids. Front. Microbiol. 2020, 11, 868. [Google Scholar] [CrossRef] [Scilit]
- Mahalle, S.; Bhende, R.S.; Bokade, P.; Bajaj, A.; Dafale, N.A. Emerging microbial remediation methods for rejuvenation of pesticide-contaminated sites. Total Environ. Microbiol. 2025, 1, 100026. [Google Scholar] [CrossRef] [Scilit]
- Dai, Y.; Li, N.; Zhao, Q.; Xie, S. Bioremediation using Novosphingobium strain DY4 for 2,4-dichlorophenoxyacetic acid-contaminated soil and impact on microbial community structure. Biodegradation 2015, 26, 161–170. [Google Scholar] [CrossRef] [Scilit]
- Amani, F.; Safari, S.A.A.; Ebrahimi, F.; Nazarian, S. Biodegradation of Chlorpyrifos and Diazinon Organophosphates by Two Bacteria Isolated from Contaminated Agricultural Soils. Biol. J. Microorg. 2019, 7, 27–39. [Google Scholar] [CrossRef] [Scilit]
- Ishag, A.E.S.A.; Abdelbagi, A.O.; Hammad, A.M.A.; Elsheikh, E.A.E.; Elsaid, O.E.; Hur, J.H. Biodegradation of endosulfan and pendimethalin by three strains of bacteria isolated from pesticides-polluted soils in the Sudan. Appl. Biol. Chem. 2017, 60, 287–297. [Google Scholar] [CrossRef] [Scilit]
- Leys, N.M.E.J.; Ryngaert, A.; Bastiaens, L.; Verstraete, W.; Top, E.M.; Springael, D. Occurrence and Phylogenetic Diversity of Sphingomonas Strains in Soils Contaminated with Polycyclic Aromatic Hydrocarbons. Appl. Environ. Microbiol. 2004, 70, 1944. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Tang, H.; Li, J.; Hu, H.; Xu, P. A newly isolated strain of Stenotrophomonas sHydrolyzes acetamiprid, a synthetic insecticide. Process Biochem. 2012, 47, 1820–1825. [Google Scholar] [CrossRef] [Scilit]
- Cycoń, M.; Mrozik, A.; Piotrowska-Seget, Z. Bioaugmentation as a strategy for the remediation of pesticide-polluted soil: A review. Chemosphere 2017, 172, 52–71. [Google Scholar] [CrossRef] [Scilit]
- Hassan, S.; Ganai, B.A. Deciphering the recent trends in pesticide bioremediation using genome editing and multi-omics approaches: A review. World J. Microbiol. Biotechnol. 2023, 39, 151. [Google Scholar] [CrossRef] [Scilit]
- Parte, S.G.; Mohekar, A.D.; Kharat, A.S. Microbial degradation of pesticide: A review. Afr. J. Microbiol. Res. 2017, 11, 992–1012. [Google Scholar] [CrossRef] [Scilit]
- Zhang, J.; Lu, L.; Chen, F.; Chen, L.; Yin, J.; Huang, X. Detoxification of diphenyl ether herbicide lactofen by Bacillus sp. Za and enantioselective characteristics of an esterase gene lacE. J. Hazard. Mater. 2018, 341, 336–345. [Google Scholar] [CrossRef] [Scilit]
- Geed, S.R.; Kureel, M.K.; Shukla, A.K.; Singh, R.S.; Rai, B.N. Biodegradation of malathion and evaluation of kinetic parameters using three bacterial species. Resour. Technol. 2016, 2, S3–S11. [Google Scholar] [CrossRef] [Scilit]
- Zhang, T.; Zhang, H. Microbial Consortia Are Needed to Degrade Soil Pollutants. Microorganisms 2022, 10, 261. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cao, Z.; Yan, W.; Ding, M.; Yuan, Y. Construction of microbial consortia for microbial degradation of complex compounds. Front. Bioeng. Biotechnol. 2022, 10, 1051233. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chaudhary, P.; Xu, M.; Ahamad, L.; Chaudhary, A.; Kumar, G.; Adeleke, B.S.; Verma, K.K.; Hu, D.-M.; Širić, I.; Kumar, P. Application of Synthetic Consortia for Improvement of Soil Fertility, Pollution Remediation, and Agricultural Productivity: A Review. Agronomy 2023, 13, 643. [Google Scholar] [CrossRef] [Scilit]
- Guo, D.D.; Luo, L.-M.; Ma, H.-L.; Zhang, S.-P.; Xu, H.; Zhang, H.; Wang, Y.; Yuan, Y.; Wang, Z.; He, Y.-X. The Regulator PltZ Regulates a Putative ABC Transporter System PltIJKNOP of Pseudomonas aeruginosa ATCC 27853 in Response to the Antimicrobial 2,4-Diacetylphloroglucinol. Front. Microbiol. 2020, 11, 1423. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dechesne, A.; Badawi, N.; Aamand, J.; Smets, B.F. Fine scale spatial variability of microbial pesticide degradation in soil: Scales, controlling factors, and implications. Front. Microbiol. 2014, 5, 667. [Google Scholar] [CrossRef] [Scilit]
- Cycoń, M.; Piotrowska-Seget, Z. Biochemical and microbial soil functioning after application of the insecticide imidacloprid. J. Environ. Sci. 2015, 27, 147–158. [Google Scholar] [CrossRef] [Scilit]
- Erguven, G.O.; Demirci, U. Using Ochrobactrum thiophenivorans and Sphingomonas melonis for bioremediation of Imidacloprid. Environ. Technol. Innov. 2021, 21, 101236. [Google Scholar] [CrossRef] [Scilit]
- Raimondo, E.E.; Aparicio, J.D.; Bigliardo, A.L.; Fuentes, M.S.; Benimeli, C.S. Enhanced bioremediation of lindane-contaminated soils through microbial bioaugmentation assisted by biostimulation with sugarcane filter cake. Ecotoxicol. Environ. Saf. 2020, 190, 110143. [Google Scholar] [CrossRef] [Scilit]
- Hou, R.; Zhang, J.; Fu, Q.; Li, T.; Gao, S.; Wang, R.; Zhao, S.; Zhu, B. The boom era of emerging contaminants: A review of remediating agricultural soils by biochar. Sci. Total Environ. 2024, 931, 172899. [Google Scholar] [CrossRef] [Scilit]
- Han, S.; Tao, Y.; Zhao, L.; Cui, Y.; Zhang, Y. Metabolic insights into how multifunctional microbial consortium enhances atrazine removal and phosphorus uptake at low temperature. J. Hazard. Mater. 2024, 461, 132539. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, W.J.; Zhang, W.; Lei, Q.; Chen, S.-F.; Huang, Y.; Bhatt, K.; Liao, L.; Zhou, X. Pseudomonas aeruginosa based concurrent degradation of beta-cypermethrin and metabolite 3-phenoxybenzaldehyde, and its bioremediation efficacy in contaminated soils. Environ. Res. 2023, 236, 116619. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sun, S.; Guo, J.; Zhu, Z.; Zhou, J. Microbial degradation mechanisms of the neonicotinoids acetamiprid and flonicamid and the associated toxicity assessments. Front. Microbiol. 2024, 15, 1500401. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wei, J.; Wang, X.; Tu, C.; Long, T.; Bu, Y.; Wang, H.; Jeyakumar, P.; Jiang, J.; Deng, S. Remediation technologies for neonicotinoids in contaminated environments: Current state and future prospects. Environ. Int. 2023, 178, 108044. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pashirova, T.; Salah-Tazdaït, R.; Tazdaït, D.; Masson, P. Applications of Microbial Organophosphate-Degrading Enzymes to Detoxification of Organophosphorous Compounds for Medical Countermeasures against Poisoning and Environmental Remediation. Int. J. Mol. Sci. 2024, 25, 7822. [Google Scholar] [CrossRef] [Scilit]
- Serdar, C.M.; Gibson, D.T. Enzymatic hydrolysis of organophosphates by a bacterial phosphotriesterase. Biotechnol. Bioeng. 1982, 24, 1473–1480. [Google Scholar] [CrossRef] [Scilit]
- Donarski, W.J.; Dumas, D.P.; Heitmeyer, D.P.; Lewis, V.E.; Raushel, F.M. Structure-Activity Relationships in the Hydrolysis of Substrates by the Phosphotriesterase from Pseudomonas diminuta. Biochemistry 1989, 28, 4650–4655. [Google Scholar] [CrossRef] [Scilit]
- Meier, M.M.; Rajendran, C.; Malisi, C.; Fox, N.G.; Xu, C.; Schlee, S.; Barondeau, D.P.; Höcker, B.; Sterner, R.; Raushel, F.M. Molecular Engineering of Organophosphate Hydrolysis Activity from a Weak Promiscuous Lactonase Template. J. Am. Chem. Soc. 2013, 135, 11670–11677. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aubert, S.D.; Li, Y.; Raushel, F.M. Mechanism for the Hydrolysis of Organophosphates by the Bacterial Phosphotriesterase†. Biochemistry 2004, 43, 5707–5715. [Google Scholar] [CrossRef] [Scilit]
- Zhang, X.; Wu, R.; Song, L.; Lin, Y.; Lin, M.; Cao, Z.; Wu, W.; Mo, Y. Molecular dynamics simulations of the detoxification of paraoxon catalyzed by phosphotriesterase. J. Comput. Chem. 2009, 30, 2388–2401. [Google Scholar] [CrossRef] [Scilit]
- Xu, J.; Wang, B.; Wang, M.-Q.; Gao, J.-J.; Li, Z.-J.; Tian, Y.-S.; Peng, R.-H.; Yao, Q.-H. Metabolic Engineering of Escherichia coli for Methyl Parathion Degradation. Front. Microbiol. 2022, 13, 679126. [Google Scholar] [CrossRef] [Scilit]
- Pande, V.; Pandey, S.C.; Sati, D.; Bhatt, P.; Samant, M. Microbial Interventions in Bioremediation of Heavy Metal Contaminants in Agroecosystem. Front. Microbiol. 2022, 13, 824084. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Aswathi, A.; Pandey, A.; Sukumaran, R.K. Rapid degradation of the organophosphate pesticide–Chlorpyrifos by a novel strain of Pseudomonas nitroreducens AR-3. Bioresour. Technol. 2019, 292, 122025. [Google Scholar] [CrossRef] [Scilit]
- Cosgrove, S.C.; Miller, G.J.; Bornadel, A.; Dominguez, B. Realizing the Continuous Chemoenzymatic Synthesis of Anilines Using an Immobilized Nitroreductase. ACS Sustain. Chem. Eng. 2023, 11, 8556–8561. [Google Scholar] [CrossRef] [Scilit]
- Gautam, P.; Dubey, S.K. Biodegradation of Neonicotinoids: Current Trenads and Future Prospects. Curr. Pollut. Reports 2023, 9, 410–432. [Google Scholar] [CrossRef] [Scilit]
- Zeng, Y.; Sun, S.; Li, P.; Zhou, X.; Wang, J. Neonicotinoid Insecticide-Degrading Bacteria and Their Application Potential in Contaminated Agricultural Soil Remediation. Agrochemicals 2024, 3, 29–41. [Google Scholar] [CrossRef] [Scilit]
- Kumar, G.; Lal, S.; Soni, S.K.; Maurya, S.K.; Shukla, P.K.; Chaudhary, P.; Bhattacherjee, A.K.; Garg, N. Mechanism and kinetics of chlorpyrifos co-metabolism by using environment restoring microbes isolated from rhizosphere of horticultural crops under subtropics. Front. Microbiol. 2022, 13, 891870. [Google Scholar] [CrossRef] [Scilit]
- Bilal, M.; Iqbal, H.M.N.; Barceló, D. Persistence of pesticides-based contaminants in the environment and their effective degradation using laccase-assisted biocatalytic systems. Sci. Total Environ. 2019, 695, 133896. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Scott, C.; Pandey, G.; Hartley, C.J.; Oakeshott, J.G. The enzymatic basis for pesticide bioremediation. Indian J. Microbiol. 2008, 48, 65–79. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Vaithyanathan, V.K.; Vaidyanathan, V.K.; Cabana, H. Laccase-Driven Transformation of High Priority Pesticides Without Redox Mediators: Towards Bioremediation of Contaminated Wastewaters. Front. Bioeng. Biotechnol. 2022, 9, 770435. [Google Scholar] [CrossRef] [Scilit]
- Hu, W.; Lu, Q.; Zhong, G.; Hu, M.; Yi, X. Biodegradation of Pyrethroids by a Hydrolyzing Carboxylesterase EstA from Bacillus cereus BCC01. Appl. Sci. 2019, 9, 477. [Google Scholar] [CrossRef] [Scilit]
- Chauhan, P.S.; Jha, B. Pilot scale production of extracellular thermo-alkali stable laccase from Pseudomonas Sp. S2 using agro waste and its application in organophosphorous pesticides degradation. J. Chem. Technol. Biotechnol. 2018, 93, 1022–1030. [Google Scholar] [CrossRef] [Scilit]
- Bhatt, P.; Huang, Y.; Zhan, H.; Chen, S. Insight into microbial applications for the biodegradation of pyrethroid insecticides. Front. Microbiol. 2019, 10, 457788. [Google Scholar] [CrossRef] [Scilit]
- Gangola, S.; Sharma, A.; Bhatt, P.; Khati, P.; Chaudhary, P. Presence of esterase and laccase in Bacillus subtilis facilitates biodegradation and detoxification of cypermethrin. Sci. Reports 2018, 8, 1–11. [Google Scholar] [CrossRef] [Scilit]
- Lv, N.; Li, R.; Cheng, S.; Zhang, L.; Liang, P.; Gao, X. The gut symbiont Sphingomonas mediates imidacloprid resistance in the important agricultural insect pest Aphis gossypii Glover. BMC Biol. 2023, 21, 86. [Google Scholar] [CrossRef] [Scilit]
- Ma, Y.; Zhai, S.; Mao, S.Y.; Sun, S.L.; Wang, Y.; Liu, Z.H.; Dai, Y.J.; Yuan, S. Co-metabolic transformation of the neonicotinoid insecticide imidacloprid by the new soil isolate Pseudoxanthomonas indica CGMCC 6648. J. Environ. Sci. Health Part B Pestic. Food Contam. Agric. Wastes 2014, 49, 661–670. [Google Scholar] [CrossRef] [Scilit]
- Sharma, N.; Zhai, S.; Mao, S.Y.; Sun, S.L.; Wang, Y.; Liu, Z.H.; Dai, Y.J.; Yuan, S. Metagenomic insights into microbial community, functional annotation, and antibiotic resistance genes in Himalayan Brahmaputra River sediment, India. Front. Microbiol. 2024, 15, 1426463. [Google Scholar] [CrossRef] [Scilit]
- Koonin, E.V.; Makarova, K.S. Origins and evolution of CRISPR-Cas systems. Philos. Trans. R. Soc. B Biol. Sci. 2019, 374, 20180087. [Google Scholar] [CrossRef] [Scilit]
- Dank, A.; Smid, E.J.; Notebaart, R.A. CRISPR-Cas genome engineering of esterase activity in Saccharomyces cerevisiae steers aroma formation. BMC Res. Notes 2018, 11, 682. [Google Scholar] [CrossRef] [Scilit]
- Eddleston, M.; Clutton, R.E.; Taylor, M.; Thompson, A.; Worek, F.; John, H.; Thiermann, H.; Scott, C. Efficacy of an organophosphorus hydrolase enzyme (OpdA) in human serum and minipig models of organophosphorus insecticide poisoning. Clin. Toxicol. 2020, 58, 397–405. [Google Scholar] [CrossRef] [Scilit]
- Khan, M.F.; Liao, J.; Liu, Z.; Chugh, G. Bacterial Cytochrome P450 Involvement in the Biodegradation of Fluorinated Pyrethroids. J. Xenobiotics 2025, 15, 58. [Google Scholar] [CrossRef] [Scilit]
- Wolfand, J.M.; Lefevre, G.H.; Luthy, R.G. Metabolization and degradation kinetics of the urban-use pesticide fipronil by white rot fungus Trametes versicolor. Environ. Sci. Process. Impacts 2016, 18, 1256–1265. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Siminszky, B. Plant cytochrome P450-mediated herbicide metabolism. Phytochem. Rev. 2006, 5, 445–458. [Google Scholar] [CrossRef] [Scilit]
- Lourthuraj, A.A.; Hatshan, M.R.; Hussein, D.S. Biocatalytic degradation of organophosphate pesticide from the wastewater and hydrolytic enzyme properties of consortium isolated from the pesticide contaminated water. Environ. Res. 2022, 205, 112553. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sirotkina, M.; Lyagin, I.; Efremenko, E. Hydrolysis of organophosphorus pesticides in soil: New opportunities with ecocompatible immobilized His6-OPH. Int. Biodeterior. Biodegrad. 2012, 68, 18–23. [Google Scholar] [CrossRef] [Scilit]
- Manikandan, S.K.; Pallavi, P.; Shetty, K.; Bhattacharjee, D.; Giannakoudakis, D.A.; Katsoyiannis, I.A.; Nair, V. Effective Usage of Biochar and Microorganisms for the Removal of Heavy Metal Ions and Pesticides. Molecules 2023, 28, 719. [Google Scholar] [CrossRef] [Scilit]
- Randhawa, J.S. Microbial-assisted remediation approach for neonicotinoids from polluted environment. Bull. Natl. Res. Cent. 2024, 48, 70. [Google Scholar] [CrossRef] [Scilit]
- Rylott, E.L.; Bruce, N.C. How Synthetic Biology Can Help Bioremediation. Curr. Opin. Chem. Biol. 2020, 58, 86–95. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Khalid, S.; Shahid, M.; Murtaza, B.; Bibi, I.; Natasha; Naeem, M.A.; Niazi, N.K. A critical review of different factors governing the fate of pesticides in soil under biochar application. Sci. Total Environ. 2020, 711, 134645. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kalia, A.; Gosal, S.K. Effect of pesticide application on soil microorganisms. Arch. Agron. Soil Sci. 2011, 57, 569–596. [Google Scholar] [CrossRef] [Scilit]
- Delcour, I.; Spanoghe, P.; Uyttendaele, M. Literature review: Impact of climate change on pesticide use. Food Res. Int. 2015, 68, 7–15. [Google Scholar] [CrossRef] [Scilit]
- Ding, W.; Zhang, Y.; Shi, S. Development and Application of CRISPR/Cas in Microbial Biotechnology. Front. Bioeng. Biotechnol. 2020, 8, 711. [Google Scholar] [CrossRef] [Scilit]
- Yasir, M.; Hossain, A.; Pratap-Singh, A. Pesticide Degradation: Impacts on Soil Fertility and Nutrient Cycling. Environments 2025, 12, 272. [Google Scholar] [CrossRef] [Scilit]
- Ćwieląg-Piasecka, I. Soil Organic Matter Composition and pH as Factors Affecting Retention of Carbaryl, Carbofuran and Metolachlor in Soil. Molecules 2023, 28, 5552. [Google Scholar] [CrossRef] [Scilit]
- Racke, K.D.; Steele, K.P.; Yoder, R.N.; Dick, W.A.; Avidov, E. Factors Affecting the Hydrolytic Degradation of Chlorpyrifos in Soil. J. Agric. Food Chem. 1996, 44, 1582–1592. [Google Scholar] [CrossRef] [Scilit]
- Wepukhulu, M.; Wachira, P.; Huria, N.; Sifuna, P.; Essuman, S.; Asamba, M. Optimization of Growth Conditions for Chlorpyrifos-Degrading Bacteria in Farm Soils in Nakuru County, Kenya. Biomed Res. Int. 2024, 2024, 1611871. [Google Scholar] [CrossRef] [Scilit]
- Paneque, P.; Gómez, I.; Parrado, J.; Orts, J.M.; Tejada, M. Effect of soil temperature and moisture on degradation of the oxyfluorfen herbicide. Cogent Food Agric. 2025, 11, 2540979. [Google Scholar] [CrossRef] [Scilit]
- Liu, P.; Wen, S.; Zhu, S.; Hu, X.; Wang, Y. Microbial Degradation of Soil Organic Pollutants: Mechanisms, Challenges, and Advances in Forest Ecosystem Management. Processes 2025, 13, 916. [Google Scholar] [CrossRef] [Scilit]
- Siddique, T.; Okeke, B.C.; Arshad, M.; Frankenberger, W.T. Temperature and pH Effects on Biodegradation of Hexachlorocyclohexane Isomers in Water and a Soil Slurry. J. Agric. Food Chem. 2002, 50, 5070–5076. [Google Scholar] [CrossRef] [Scilit]
- Singh, B.K.; Walker, A.; Morgan, J.A.W.; Wright, D.J. Effects of Soil pH on the Biodegradation of Chlorpyrifos and Isolation of a Chlorpyrifos-Degrading Bacterium. Appl. Environ. Microbiol. 2003, 69, 5198. [Google Scholar] [CrossRef] [Scilit]
- Parven, A.; Meftaul, I.M.; Venkateswarlu, K.; Megharaj, M. Pre-emergence herbicides used in urban and agricultural settings: Dissipation and ecological implications. Environ. Geochem. Health 2024, 46, 493. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Jaikaew, P.; Malhat, F.; Boulange, J.; Watanabe, H. Aspect of the degradation and adsorption kinetics of atrazine and metolachlor in andisol soil. Hell. Plant Prot. J. 2017, 10, 1–14. [Google Scholar] [CrossRef] [Scilit]
- Książek-Trela, P.; Potocki, L.; Szpyrka, E. The impact of novel bacterial strains and their consortium on diflufenican degradation in the mineral medium and soil. Sci. Rep. 2025, 15, 18051. [Google Scholar] [CrossRef] [Scilit]
- Katagi, T. Aerobic microbial transformation of pesticides in surface water. J. Pestic. Sci. 2013, 38, 10–26. [Google Scholar] [CrossRef] [Scilit]
- Schroll, R.; Becher, H.H.; Dörfler, U.; Gayler, S.; Grundmann, S.; Hartmann, H.P.; Ruoss, J. Quantifying the effect of soil moisture on the aerobic microbial mineralization of selected pesticides in different soils. Environ. Sci. Technol. 2006, 40, 3305–3312. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Wirsching, J.; Chavez Rodriguez, L.; Ditterich, F.; Pagel, H.; He, R.; Uksa, M.; Zwiener, C.; Kandeler, E.; Poll, C. Temperature and soil moisture change microbial allocation of pesticide-derived carbon. Eur. J. Soil Sci. 2023, 74, e13417. [Google Scholar] [CrossRef] [Scilit]
- Nandi, R.; Sarker, A.; Rana, M.M.; Hasan, A.K. Influence of Organic Matter and Growing Conditions on Dissipation Behavior and Mobility of Two Pesticides in Soils. Environments 2025, 12, 123. [Google Scholar] [CrossRef] [Scilit]
- Novotny, E.H.; Turetta, A.P.D.; Resende, M.F.; Rebello, C.M. The quality of soil organic matter, accessed by 13C solid state nuclear magnetic resonance, is just as important as its content concerning pesticide sorption. Environ. Pollut. 2020, 266, 115298. [Google Scholar] [CrossRef] [Scilit]
- Rohilla, Y.; Pai, A.; Pandit, S.; Priya, K.; Ranjan, N.; Sharma, K.; Verma, R.; Nag, M.; Lahiri, D.; Bhattacharya, D. A concise review on microbial degradation of pesticides and organohalogen compounds: Recent advances and current challenges. Vegetos 2025, 1–17. [Google Scholar] [CrossRef] [Scilit]
- Ukalska-Jaruga, A.; Bejger, R.; Smreczak, B.; Weber, J.; Mielnik, L.; Jerzykiewicz, M.; Ćwieląg-Piasecka, I.; Jamroz, E.; Debicka, M.; Kocowicz, A.; et al. The Interaction of Pesticides with Humin Fractions and Their Potential Impact on Non-Extractable Residue Formation. Molecules 2023, 28, 7146. [Google Scholar] [CrossRef] [Scilit]
- Meftaul, I.M.; Venkateswarlu, K.; Annamalai, P.; Parven, A.; Megharaj, M. Degradation of four pesticides in five urban landscape soils: Human and environmental health risk assessment. Environ. Geochem. Health 2022, 45, 1599–1614. [Google Scholar] [CrossRef] [Scilit]
- Itoh, H.; Navarro, R.; Takeshita, K.; Tago, K.; Hayatsu, M.; Hori, T.; Kikuchi, Y. Bacterial population succession and adaptation affected by insecticide application and soil spraying history. Front. Microbiol. 2014, 5, 457. [Google Scholar] [CrossRef] [Scilit]
- Estop-Aragonés, C.; Knorr, K.H.; Blodau, C. Controls on in situ oxygen and dissolved inorganic carbon dynamics in peats of a temperate fen. J. Geophys. Res. Biogeosci. 2012, 117. [Google Scholar] [CrossRef] [Scilit]
- Zawierucha, I.; Malina, G. Effects of oxygen supply on the biodegradation rate in oil hydrocarbons contaminated soil. J. Phys. Conf. Ser. 2011, 289, 12035. [Google Scholar] [CrossRef] [Scilit]
- Richard, T.L.; Veeken, A.H.M.; De Wilde, V.; Hamelers, H.V.M. Air-Filled Porosity and Permeability Relationships during Solid-State Fermentation. Biotechnol. Prog. 2004, 20, 1372–1381. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chowdhury, I.F.; Doran, G.S.; Stodart, B.J.; Chen, C.; Wu, H. Microbial Degradation of Herbicide Residues in Australian Soil: An Overview of Mechanistic Insights and Recent Advancements. Toxics 2025, 13, 949. [Google Scholar] [CrossRef] [Scilit]
- Kanissery, R.; Liu, W.; Tiwari, R.; Sims, G. Impact of Soil Aeration on the Environmental Fate of Pre-Emergent Herbicide Metolachlor. Appl. Sci. 2021, 11, 8567. [Google Scholar] [CrossRef] [Scilit]
- Schwarz, E.; Khurana, S.; Chakrawal, A.; Chavez Rodriguez, L.; Wirsching, J.; Streck, T.; Manzoni, S.; Thullner, M.; Pagel, H. Spatial Control of Microbial Pesticide Degradation in Soil: A Model-Based Scenario Analysis. Environ. Sci. Technol. 2022, 56, 14427–14438. [Google Scholar] [CrossRef] [Scilit]
- Ewere, E.E.; White, S.; Mauleon, R.; Benkendorff, K. Soil microbial communities and degradation of pesticides in greenhouse effluent through a woodchip bioreactor. Environ. Pollut. 2024, 359, 124561. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Kumar, S.; Anshumali. Biogeochemical appraisal of carbon fractions and carbon stock in riparian soils of the Ganga River basin. Appl. Soil Ecol. 2023, 182, 104687. [Google Scholar] [CrossRef] [Scilit]
- Qattan, S.Y.A. Harnessing bacterial consortia for effective bioremediation: Targeted removal of heavy metals, hydrocarbons, and persistent pollutants. Environ. Sci. Eur. 2025, 371, 37. [Google Scholar] [CrossRef] [Scilit]
- Varjani, S.; Kumar, G.; Rene, E.R. Developments in biochar application for pesticide remediation: Current knowledge and future research directions. J. Environ. Manag. 2019, 232, 505–513. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cara, I.G.; Țopa, D.; Puiu, I.; Jităreanu, G. Biochar a Promising Strategy for Pesticide-Contaminated Soils. Agriculture 2022, 12, 1579. [Google Scholar] [CrossRef] [Scilit]
- De Silva, S.; Gamage, L.K.H.; Thapa, V.R. Impact of Drought on Soil Microbial Communities. Microorganisms 2025, 13, 1625. [Google Scholar] [CrossRef] [Scilit]
- Zhelezova, A.; Cederlund, H.; Stenström, J. Effect of Biochar Amendment and Ageing on Adsorption and Degradation of Two Herbicides. Water Air. Soil Pollut. 2017, 228, 216. [Google Scholar] [CrossRef] [Scilit]
- Zhang, C.; Hu, X.; Luo, J.; Wu, Z.; Wang, L.; Li, B.; Wang, Y.; Sun, G. Degradation dynamics of glyphosate in different types of citrus orchard soils in China. Molecules 2015, 20, 1161–1175. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sun, C.; Liu, Y.; Bei, K.; Zheng, W.; Wang, Q.; Wang, Q. Impact of biochar on the degradation rates of three pesticides by vegetables and its effects on soil bacterial communities under greenhouse conditions. Sci. Rep. 2024, 14, 19986. [Google Scholar] [CrossRef] [Scilit]
- Jayasekara, S.K.; Ratnayake, R.R. The bioremediation of agricultural soils polluted with pesticides. In Microbial Syntrophy-Mediated Eco-Enterprising; Academic Press: New York, NY, USA, 2022; pp. 15–39. [Google Scholar] [CrossRef] [Scilit]
- Raffa, C.M.; Chiampo, F. Bioremediation of Agricultural Soils Polluted with Pesticides: A Review. Bioengineering 2021, 8, 92. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Cabrera, S.; Zubillaga, M.; Montserrat, J.M. Natural attenuation and bioremediation of chlorpyrifos and endosulfan in periurban horticultural soils of Buenos Aires (Argentina) using microcosms assays. Appl. Soil Ecol. 2022, 169, 104192. [Google Scholar] [CrossRef] [Scilit]
- Gonçalves, C.R.; da Silva Delabona, P. Strategies for bioremediation of pesticides: Challenges and perspectives of the Brazilian scenario for global application–A review. Environ. Adv. 2022, 8, 100220. [Google Scholar] [CrossRef] [Scilit]
- Villaverde, J.; Rubio-Bellido, M.; Lara-Moreno, A.; Merchan, F.; Morillo, E. Combined use of microbial consortia isolated from different agricultural soils and cyclodextrin as a bioremediation technique for herbicide contaminated soils. Chemosphere 2018, 193, 118–125. [Google Scholar] [CrossRef] [Scilit]
- Ruan, Z.; Chen, K.; Cao, W.; Meng, L.; Yang, B.; Xu, M.; Xing, Y.; Li, P.; Freilich, S.; Chen, C.; et al. Engineering natural microbiomes toward enhanced bioremediation by microbiome modeling. Nat. Commun. 2024, 15, 4694. [Google Scholar] [CrossRef] [Scilit]
- Shahid, M.; Khan, M.S.; Singh, U.B. Pesticide-tolerant microbial consortia: Potential candidates for remediation/clean-up of pesticide-contaminated agricultural soil. Environ. Res. 2023, 236, 116724. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Coppola, L.; Castillo, M.D.P.; Monaci, E.; Vischetti, C. Adaptation of the Biobed Composition for Chlorpyrifos Degradation to Southern Europe Conditions. J. Agric. Food Chem. 2006, 55, 396–401. [Google Scholar] [CrossRef] [Scilit]
- Tortella, G.R.; Rubilar, O.; Castillo, M.D.P.; Cea, M.; Mella-Herrera, R.; Diez, M.C. Chlorpyrifos degradation in a biomixture of biobed at different maturity stages. Chemosphere 2012, 88, 224–228. [Google Scholar] [CrossRef] [Scilit]
- Singh, R.P.; Yadav, R.; Pandey, V.; Singh, A.; Singh, M.; Shanker, K.; Khare, P. Effect of biochar on soil microbial community, dissipation and uptake of chlorpyrifos and atrazine. Biochar 2024, 6, 1–17. [Google Scholar] [CrossRef] [Scilit]
- Mussali-Galante, P.; Castrejón-Godínez, M.L.; Díaz-Soto, J.A.; Vargas-Orozco, Á.P.; Quiroz-Medina, H.M.; Tovar-Sánchez, E.; Rodríguez, A. Biobeds, a Microbial-Based Remediation System for the Effective Treatment of Pesticide Residues in Agriculture. Agriculture 2023, 13, 1289. [Google Scholar] [CrossRef] [Scilit]
- Spliid, N.H.; Helweg, A.; Heinrichson, K. Leaching and degradation of 21 pesticides in a full-scale model biobed. Chemosphere 2006, 65, 2223–2232. [Google Scholar] [CrossRef] [Scilit]
- Cooper, R.J.; Fitt, P.; Hiscock, K.M.; Lovett, A.A.; Gumm, L.; Dugdale, S.J.; Rambohul, J.; Williamson, A.; Noble, L.; Beamish, J.; et al. Assessing the effectiveness of a three-stage on-farm biobed in treating pesticide contaminated wastewater. J. Environ. Manag. 2016, 181, 874–882. [Google Scholar] [CrossRef] [Scilit]
- Góngora-Echeverría, V.R.; Quintal-Franco, C.; Arena-Ortiz, M.L.; Giácoman-Vallejos, G.; Ponce-Caballero, C. Identification of microbial species present in a pesticide dissipation process in biobed systems using typical substrates from southeastern Mexico as a biomixture at a laboratory scale. Sci. Total Environ. 2018, 628–629, 528–538. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Góngora-Echeverría, V.R.; Martin-Laurent, F.; Quintal-Franco, C.; Giácoman-Vallejos, G.; Ponce-Caballero, C. Agricultural effluent treatment in biobed systems using novel substrates from southeastern Mexico: The relationship with physicochemical parameters of biomixtures. Environ. Sci. Pollut. Res. 2017, 24, 9741–9753. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Domínguez-Rodríguez, V.I.; Baltierra-Trejo, E.; Gómez-Cruz, R.; Adams, R.H. Microbial growth in biobeds for treatment of residual pesticide in banana plantations. PeerJ 2021, 9, e12200. [Google Scholar] [CrossRef] [Scilit]
- de A., L.; Gebler, L.; Niemeyer, J.C.; Itako, A.T. Destination of pesticide residues on biobeds: State of the art and future perspectives in Latin America. Chemosphere 2020, 248, 126038. [Google Scholar] [CrossRef] [Scilit]
- Feng, S.; Khurana, S.; Chakrawal, A.; Chavez Rodriguez, L.; Wirsching, J.; Streck, T.; Manzoni, S.; Thullner, M.; Pagel, H. Bioaugmentation potential evaluation of a bacterial consortium composed of isolated Pseudomonas and Rhodococcus for degrading benzene, toluene and styrene in sludge and sewage. Bioresour. Technol. 2021, 320, 124329. [Google Scholar] [CrossRef] [Scilit]
- Singh, D.K. Biodegradation and bioremediation of pesticide in soil: Concept, method and recent developments. Indian J. Microbiol. 2008, 48, 35–40. [Google Scholar] [CrossRef] [Scilit]
- Silva, E.; Fialho, A.M.; Sa-Correia, I.; Burns, R.G.; Shaw, L.J. Combined Bioaugmentation and Biostimulation to Cleanup Soil Contaminated with High Concentrations of Atrazine. Environ. Sci. Technol. 2003, 38, 632–637. [Google Scholar] [CrossRef] [Scilit]
- Arriagada-Escamilla, C.; Alvarado, R.; Ortiz, J.; Campos-Vargas, R.; Cornejo, P. Alginate–Bentonite Encapsulation of Extremophillic Bacterial Consortia Enhances Chenopodium quinoa Tolerance to Metal Stress. Microorganisms 2024, 12, 2066. [Google Scholar] [CrossRef] [Scilit]
- Balla, A.; Silini, A.; Cherif-Silini, H.; Mapelli, F.; Borin, S. Root colonization dynamics of alginate encapsulated rhizobacteria: Implications for Arabidopsis thaliana root growth and durum wheat performance. AIMS Microbiol. 2025, 11, 87. [Google Scholar] [CrossRef] [Scilit]
- Peng, T.; Huang, Y.; Yang, T.; Wang, Y.; Jin, L. Enhanced phoxim biodegradation by immobilizing Novosphingobium Sp. RL4 on attapulgite-sodium alginate. Front. Microbiol. 2025, 16, 1541328. [Google Scholar] [CrossRef] [Scilit]
- Sharma, S.; Singh, B.; Gupta, V.K. Biodegradation of imidacloprid by consortium of two soil isolated bacillus sp. Bull. Environ. Contam. Toxicol. 2014, 93, 637–642. [Google Scholar] [CrossRef] [Scilit]
- Talpur, F.N.; Unar, A.; Bhatti, S.K.; Alsawalha, L.; Fouad, D.; Bashir, H.; Afridi, H.I.; Ataya, F.S.; Jefri, O.A.; Bashir, M.S. Bioremediation of Neonicotinoid Pesticide, Imidacloprid, Mediated by Bacillus cereus. Bioengineering 2023, 10, 951. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shi, G.; Li, H.; Fu, Q.; Li, T.; Hou, R.; Chen, Q.; Xue, P. Effects of biochar and compost on the abundant and rare microbial communities assembly and multifunctionality in pesticide-contaminated soil under freeze–thaw cycles. Environ. Pollut. 2024, 362, 125003. [Google Scholar] [CrossRef] [Scilit]
- Tang, X.; Zheng, W.; Chen, L.; Liu, H.; Li, M.; Chen, M.; Yang, Y. Enhancing neonicotinoid removal in recirculating constructed wetlands: The impact of Fe/Mn biochar and microbial interactions. J. Hazard. Mater. 2024, 476, 135139. [Google Scholar] [CrossRef] [Scilit]
- Rafeeq, H.; Afsheen, N.; Rafique, S.; Arshad, A.; Intisar, M.; Hussain, A.; Bilal, M.; Iqbal, H.M.N. Genetically engineered microorganisms for environmental remediation. Chemosphere 2023, 310, 136751. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Shi, G.; Hou, R.; Fu, Q.; Li, T.; Chen, Q. Effects of biochar and compost on microbial community assembly and metabolic processes in glyphosate, imidacloprid and pyraclostrobin polluted soil under freezethaw cycles. J. Hazard. Mater. 2024, 471, 134397. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sethi, G.; Saini, R.; Banerjee, T.; Singh, N. Bioaugmentation: A strategy for enhanced degradation of pesticides in biobed. J. Environ. Sci. Health Part B Pestic. Food Contam. Agric. Wastes 2024, 59, 654–662. [Google Scholar] [CrossRef] [Scilit]
- Zhang, M.; Li, Q.; Bai, X.; Gao, S.; Zhu, Q.; Ye, B.; Zhou, Y.; Qiu, J.; Yan, X.; Hong, Q. Construction of an Unmarked Genetically Engineered Strain Bacillus subtilis Wb800-Ipah and its Pilot Application. SSRN Electron. J. 2023, 176, 105527. [Google Scholar] [CrossRef] [Scilit]
- Meng, C.; He, Q.; Huang, J.-W.; Cao, Q.; Yan, X.; Li, S.-P.; Jiang, J.-D. Degradation of chlorothalonil through a hydrolytic dehalogenase secreted from Bacillus subtilis WB800. Int. Biodeterior. Biodegrad. 2015, 104, 97–104. [Google Scholar] [CrossRef] [Scilit]
- Ye, B.; Luo, Y.; Zhong, B.; Zhu, J.; Huang, J.; Gu, J.; Jiang, J.; Yan, X.; He, J.; He, Q. High-level stable expression of gene for preparation of chlorothalonil hydrolytic dehalogenase and its application in elimination of chlorothalonil inhibition on bioconversion of lignocellulosic biomass. J. Biosci. Bioeng. 2020, 130, 630–636. [Google Scholar] [CrossRef] [Scilit]
- Morillo, E.; Madrid, F.; Lara-Moreno, A.; Villaverde, J. Soil bioremediation by cyclodextrins. A review. Int. J. Pharm. 2020, 591, 119943. [Google Scholar] [CrossRef] [Scilit]
- Anwar, S.; Liaqat, A.; Munir, A.; Ashraf, M.F.; Iqbal, S. Bioaugmentation of a novel bacterial consortium in cotton-planted soil for lambda-cyhalothrin degradation. Pedosphere 2024, 34, 1100–1110. [Google Scholar] [CrossRef] [Scilit]
- Faridy, N.; Torabi, E.; Pourbabaee, A.A.; Osdaghi, E.; Talebi, K. Efficacy of novel bacterial consortia in degrading fipronil and thiobencarb in paddy soil: A survey for community structure and metabolic pathways. Front. Microbiol. 2024, 15, 1366951. [Google Scholar] [CrossRef] [Scilit]
- Duncker, K.E.; Holmes, Z.A.; You, L. Engineered microbial consortia: Strategies and applications. Microb. Cell Factories 2021, 20, 211. [Google Scholar] [CrossRef] [Scilit]
- Nies, D.H. Efflux-mediated heavy metal resistance in prokaryotes. FEMS Microbiol. Rev. 2003, 27, 313–339. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Stirling, F.; Naydich, A.; Bramante, J.; Barocio, R.; Certo, M.; Wellington, H.; Redfield, E.; O’Keefe, S.; Gao, S.; Cusolito, A.; et al. Synthetic Cassettes for pH-Mediated Sensing, Counting, and Containment. Cell Rep. 2020, 30, 3139–3148.e4. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Malla, M.A.; Dubey, A.; Raj, A.; Kumar, A.; Upadhyay, N.; Yadav, S. Emerging frontiers in microbe-mediated pesticide remediation: Unveiling role of omics and In silico approaches in engineered environment. Environ. Pollut. 2022, 299, 118851. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pino, N.; Peñuela, G. Simultaneous degradation of the pesticides methyl parathion and chlorpyrifos by an isolated bacterial consortium from a contaminated site. Int. Biodeterior. Biodegrad. 2011, 65, 827–831. [Google Scholar] [CrossRef] [Scilit]
- Stirling, F.; Bitzan, L.; O’Keefe, S.; Redfield, E.; Oliver, J.W.K.; Way, J.; Silver, P.A. Rational Design of Evolutionarily Stable Microbial Kill Switches. Mol. Cell 2017, 68, 686–697.e3. [Google Scholar] [CrossRef] [Scilit]
- Yameen, M.Z.; Naqvi, S.R.; Juchelková, D.; Khan, M.N.A. Harnessing the power of functionalized biochar: Progress, challenges, and future perspectives in energy, water treatment, and environmental sustainability. Biochar 2024, 6, 25. [Google Scholar] [CrossRef] [Scilit]
- Castillo, M.D.P.; Torstensson, L.; Stenström, J. Biobeds for Environmental Protection from Pesticide Use–A Review. J. Agric. Food Chem. 2008, 56, 6206–6219. [Google Scholar] [CrossRef] [Scilit]
- Fogg, P.; Boxall, A.B.A.; Walker, A.; Jukes, A.A. Pesticide degradation in a ‘biobed’ composting substrate. Pest Manag. Sci. 2003, 59, 527–537. [Google Scholar] [CrossRef] [Scilit]
- Guo, Z.; Zhou, H.; Yin, H.; Wei, X.; Dang, Z. Functional bacterial consortium responses to biochar and implications for BDE-47 transformation: Performance, metabolism, community assembly and microbial interaction. Environ. Pollut. 2022, 313, 120120. [Google Scholar] [CrossRef] [Scilit]
- Xiang, L.; Harindintwali, J.D.; Wang, F.; Redmile-Gordon, M.; Chang, S.X.; Fu, Y.; He, C.; Muhoza, B.; Brahushi, F.; Bolan, N.; et al. Integrating Biochar, Bacteria, and Plants for Sustainable Remediation of Soils Contaminated with Organic Pollutants. Environ. Sci. Technol. 2022, 56, 16546–16566. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Mukherjee, S.; Sarkar, B.; Aralappanavar, V.K.; Mukhopadhyay, R.; Basak, B.B.; Srivastava, P.; Marchut-Mikołajczyk, O.; Bhatnagar, A.; Semple, K.T.; Bolan, N. Biochar-microorganism interactions for organic pollutant remediation: Challenges and perspectives. Environ. Pollut. 2022, 308, 119609. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Dias, L.A.; Itako, A.T.; Gebler, L.; Tolentino Júnior, J.B.; Pizzutti, I.R.; Fontana, M.E.; Janisch, B.D.; Niemeyer, J.C. Pine Litter and Vermicompost as Alternative Substrates for Biobeds: Efficiency in Pesticide Degradation. Water. Air. Soil Pollut. 2021, 232, 283. [Google Scholar] [CrossRef] [Scilit]
- Acosta-Sánchez, A.; Soto-Garita, C.; Masís-Mora, M.; Cambronero-Heinrichs, J.C.; Rodríguez-Rodríguez, C.E. Impaired pesticide removal and detoxification by biomixtures during the simulated pesticide application cycle of a tropical agricultural system. Ecotoxicol. Environ. Saf. 2020, 195, 110460. [Google Scholar] [CrossRef] [Scilit]
- Gong, T.; Xu, X.; Dang, Y.; Kong, A.; Wu, Y.; Liang, P.; Wang, S.; Yu, H.; Xu, P.; Yang, C. An engineered Pseudomonas putida can simultaneously degrade organophosphates, pyrethroids and carbamates. Sci. Total Environ. 2018, 628–629, 1258–1265. [Google Scholar] [CrossRef] [Scilit]
- Wang, H.; Su, Z.; Ren, S.; Zhang, P.; Li, H.; Guo, X.; Liu, L. Combined Use of Biochar and Microbial Agents Can Promote Lignocellulosic Degradation Microbial Community Optimization during Composting of Submerged Plants. Fermentation 2024, 10, 70. [Google Scholar] [CrossRef] [Scilit]
- Dong, M.; He, L.; Jiang, M.; Zhu, Y.; Wang, J.; Gustave, W.; Wang, S.; Deng, Y.; Zhang, X.; Wang, Z. Biochar for the Removal of Emerging Pollutants from Aquatic Systems: A Review. Int. J. Environ. Res. Public Health 2023, 20, 1679. [Google Scholar] [CrossRef] [Scilit]
- Giri, B.S.; Geed, S.; Vikrant, K.; Lee, S.S.; Kim, K.-H.; Kailasa, S.K.; Vithanage, M.; Chaturvedi, P.; Rai, B.N.; Singh, R.S. Progress in bioremediation of pesticide residues in the environment. Environ. Eng. Res. 2021, 26, 200446. [Google Scholar] [CrossRef] [Scilit]
- Sharma, P.; Singh, S.P.; Iqbal, H.M.N.; Tong, Y.W. Omics approaches in bioremediation of environmental contaminants: An integrated approach for environmental safety and sustainability. Environ. Res. 2022, 211, 113102. [Google Scholar] [CrossRef] [Scilit]
- Jaiswal, S.; Shukla, P. Alternative Strategies for Microbial Remediation of Pollutants via Synthetic Biology. Front. Microbiol. 2020, 11, 808. [Google Scholar] [CrossRef] [Scilit]
- Jeffries, T.C.; Rayu, S.; Nielsen, U.N.; Lai, K.; Ijaz, A.; Nazaries, L.; Singh, B.K. Metagenomic functional potential predicts degradation rates of a model organophosphorus xenobiotic in pesticide contaminated soils. Front. Microbiol. 2018, 9, 309432. [Google Scholar] [CrossRef] [Scilit]
- Asamba, M.N.; Mugendi, E.N.; Oshule, P.S.; Essuman, S.; Chimbevo, L.M.; Atego, N.A. Molecular characterization of chlorpyrifos degrading bacteria isolated from contaminated dairy farm soils in Nakuru County, Kenya. Heliyon 2022, 8, e09176. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Malla, M.A.; Dubey, A.; Kumar, A.; Yadav, S. Metagenomic analysis displays the potential predictive biodegradation pathways of the persistent pesticides in agricultural soil with a long record of pesticide usage. Microbiol. Res. 2022, 261, 127081. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Deng, S.; Chen, Y.; Wang, D.; Shi, T.; Wu, X.; Ma, X.; Li, X.; Hua, R.; Tang, X.; Li, Q.X. Rapid biodegradation of organophosphorus pesticides by Stenotrophomonas sp. G1. J. Hazard. Mater. 2015, 297, 17–24. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Anwar, S.; Liaquat, F.; Khan, Q.M.; Khalid, Z.M.; Iqbal, S. Biodegradation of chlorpyrifos and its hydrolysis product 3,5,6-trichloro-2-pyridinol by Bacillus pumilus strain C2A1. J. Hazard. Mater. 2009, 168, 400–405. [Google Scholar] [CrossRef] [Scilit]
- Picard, M.; Scott-Boyer, M.P.; Bodein, A.; Périn, O.; Droit, A. Integration strategies of multi-omics data for machine learning analysis. Comput. Struct. Biotechnol. J. 2021, 19, 3735–3746. [Google Scholar] [CrossRef] [Scilit]
- Renganathan, P.; Gaysina, L.A.; Gutiérrez, C.G.; Puente, E.O.R.; Sainz-Hernández, J.C. Harnessing Engineered Microbial Consortia for Xenobiotic Bioremediation: Integrating Multi-Omics and AI for Next-Generation Wastewater Treatment. J. Xenobiotics 2025, 15, 133. [Google Scholar] [CrossRef] [Scilit]
- Alidoosti, F.; Giyahchi, M.; Moien, S.; Moghimi, H. Unlocking the potential of soil microbial communities for bioremediation of emerging organic contaminants: Omics-based approaches. Microb. Cell Factories 2024, 23, 210. [Google Scholar] [CrossRef] [Scilit]
- Sun, J.; Wang, Q.; Jiang, Y.; Wen, Z.; Yang, L.; Wu, J.; Yang, S. Genome editing and transcriptional repression in Pseudomonas putida KT2440 via the type II CRISPR system. Microb. Cell Fact. 2018, 17, 41. [Google Scholar] [CrossRef] [Scilit]
- Yang, J.; Liu, R.; Song, W.; Yang, Y.; Cui, F.; Qiao, C. Construction of a genetically engineered microorganism that simultaneously degrades organochlorine and organophosphate pesticides. Appl. Biochem. Biotechnol. 2012, 166, 590–598. [Google Scholar] [CrossRef] [Scilit]
- Liu, Y.; Wang, X.; Nong, S.; Bai, Z.; Han, N.; Wu, Q.; Huang, Z.; Ding, J. Display of a novel carboxylesterase CarCby on Escherichia coli cell surface for carbaryl pesticide bioremediation. Microb. Cell Fact. 2022, 21, 97. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Chen, C.; Wang, M.; Zhu, J.; Tang, Y.; Zhang, H.; Zhao, Q.; Jing, M.; Chen, Y.; Xu, X.; Jiang, J.; et al. Long-term effect of epigenetic modification in plant–microbe interactions: Modification of DNA methylation induced by plant growth-promoting bacteria mediates promotion process. Microbiome 2022, 10, 36. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Sousa, J.F.; Amaro, H.M.; Ribeirinho-Soares, S.; Esteves, A.F.; Salgado, E.M.; Nunes, O.C.; Pires, J.C.M. Native Microalgae-Bacteria Consortia: A Sustainable Approach for Effective Urban Wastewater Bioremediation and Disinfection. Microorganisms 2024, 12, 1421. [Google Scholar] [CrossRef] [Scilit]
- Ni, H.; Li, N.; Qian, M.; He, J.; Chen, Q.; Huang, Y.; Zou, L.; Long, Z.-E.; Wang, F. Identification of a Novel Nitroreductase LNR and Its Role in Pendimethalin Catabolism in Bacillus subtilis Y3. J. Agric. Food Chem. 2019, 67, 12816–12823. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Oruganti, R.K.; Katam, K.; Show, P.L.; Gadhamshetty, V.; Upadhyayula, V.K.K.; Bhattacharyya, D. A comprehensive review on the use of algal-bacterial systems for wastewater treatment with emphasis on nutrient and micropollutant removal. Bioengineered 2022, 13, 10412–10453. [Google Scholar] [CrossRef] [Scilit]
- Ni, H.Y.; Wang, F.; Li, N.; Yao, L.; Dai, C.; He, Q.; He, J.; Hong, Q. Pendimethalin nitroreductase is responsible for the initial pendimethalin degradation step in Bacillus subtilis Y3. Appl. Environ. Microbiol. 2016, 82, 7052–7062. [Google Scholar] [CrossRef] [Scilit]
- Li, X.; Wu, S.; Dong, Y.; Fan, H.; Bai, Z.; Zhuang, X. Engineering Microbial Consortia towards Bioremediation. Water 2021, 13, 2928. [Google Scholar] [CrossRef] [Scilit]
- Lensch, A.; Abbas Lindfors, H.; Duwenig, E.; Fleischmann, T.; Hjort, C.; Kärenlampi, S.O.; McMurtry, L.; Melton, E.-D.; Andersen, M.R.; Skinner, R.; et al. Safety aspects of microorganisms deliberately released into the environment. EFB Bioecon. J. 2024, 4, 100061. [Google Scholar] [CrossRef] [Scilit]
- Kumar, N.M.; Muthukumaran, C.; Sharmila, G.; Gurunathan, B. Genetically Modified Organisms and Its Impact on the Enhancement of Bioremediation. In Bioremediation: Applications for Environmental Protection and Management; Springer: Singapore, 2018; pp. 53–76. [Google Scholar] [CrossRef] [Scilit]
- Bilal, M.; Iqbal, H.M.N. Microbial bioremediation as a robust process to mitigate pollutants of environmental concern. Case Stud. Chem. Environ. Eng. 2020, 2, 100011. [Google Scholar] [CrossRef] [Scilit]
- Orellana, R.; Cumsille, A.; Piña-Gangas, P.; Rojas, C.; Arancibia, A.; Donghi, S.; Stuardo, C.; Cabrera, P.; Arancibia, G.; Cárdenas, F.; et al. Economic Evaluation of Bioremediation of Hydrocarbon-Contaminated Urban Soils in Chile. Sustainability 2022, 14, 11854. [Google Scholar] [CrossRef] [Scilit]
- O’Brien, R.M.; Phelan, T.J.; Smith, N.M.; Smits, K.M. Remediation in developing countries: A review of previously implemented projects and analysis of stakeholder participation efforts. Crit. Rev. Environ. Sci. Technol. 2021, 51, 1259–1280. [Google Scholar] [CrossRef] [Scilit]
- Verma, J.P.; Jaiswal, D.K.; Sagar, R. Pesticide Relevance and Their Microbial Degradation: A-State-of-Art. Rev. Environ. Sci. Bio/Technology 2014, 13, 429–466. [Google Scholar] [CrossRef] [Scilit]
- Li, Z.; Fantke, P. Toward harmonizing global pesticide regulations for surface freshwaters in support of protecting human health. J. Environ. Manag. 2022, 301, 113909. [Google Scholar] [CrossRef] [Scilit]
- Michael-Igolima, U.; Abbey, S.J.; Ifelebuegu, A.O. A systematic review on the effectiveness of remediation methods for oil contaminated soils. Environ. Adv. 2022, 9, 100319. [Google Scholar] [CrossRef] [Scilit]
- Sehrawat, A.; Phour, M.; Kumar, R.; Sindhu, S.S. Bioremediation of Pesticides: An Eco-Friendly Approach for Environment Sustainability. Microorg. Sustain. 2021, 25, 23–84. [Google Scholar] [CrossRef] [Scilit]
- Pretty, J.; Bharucha, Z. Sustainable intensification in agricultural systems. Ann. Bot. 2014, 114, 1571–1596. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Nadarajah, K.; Rahman, N.S.N.A. The Microbial Connection to Sustainable Agriculture. Plants 2023, 12, 2307. [Google Scholar] [CrossRef] [Scilit]
- Aliste, M.; Ros, C.; Garrido, I.; Martínez, C.M.; Vera, A.; Siles, J.; Contreras, F.; Flores, P.; Hellín, P.; Fenoll, J.; et al. Green Manure from Cover Crops Enhances Pesticide Degradation and Soil Biological Health. J. Hazard. Mater. 2025, 495, 138984. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Bala, S.; Garg, D.; Thirumalesh, B.V.; Sharma, M.; Sridhar, K.; Inbaraj, B.S.; Tripathi, M. Recent Strategies for Bioremediation of Emerging Pollutants: A Review for a Green and Sustainable Environment. Toxics 2022, 10, 484. [Google Scholar] [CrossRef] [Scilit] [PubMed]
- Pathak, V.M.; Verma, V.K.; Rawat, B.S.; Kaur, B.; Babu, N.; Sharma, A.; Dewali, S.; Yadav, M.; Kumari, R.; Singh, S.; et al. Current status of pesticide effects on environment, human health and it’s eco-friendly management as bioremediation: A comprehensive review. Front. Microbiol. 2022, 13, 962619. [Google Scholar] [CrossRef] [Scilit]
- Osburn, E.D.; Yang, G.; Rillig, M.C.; Strickland, M.S. Evaluating the role of bacterial diversity in supporting soil ecosystem functions under anthropogenic stress. ISME Commun. 2023, 3, 66. [Google Scholar] [CrossRef] [Scilit]
| Enzyme Class | Pesticide Type | Mechanism | Bacterial Examples | Sources |
|---|---|---|---|---|
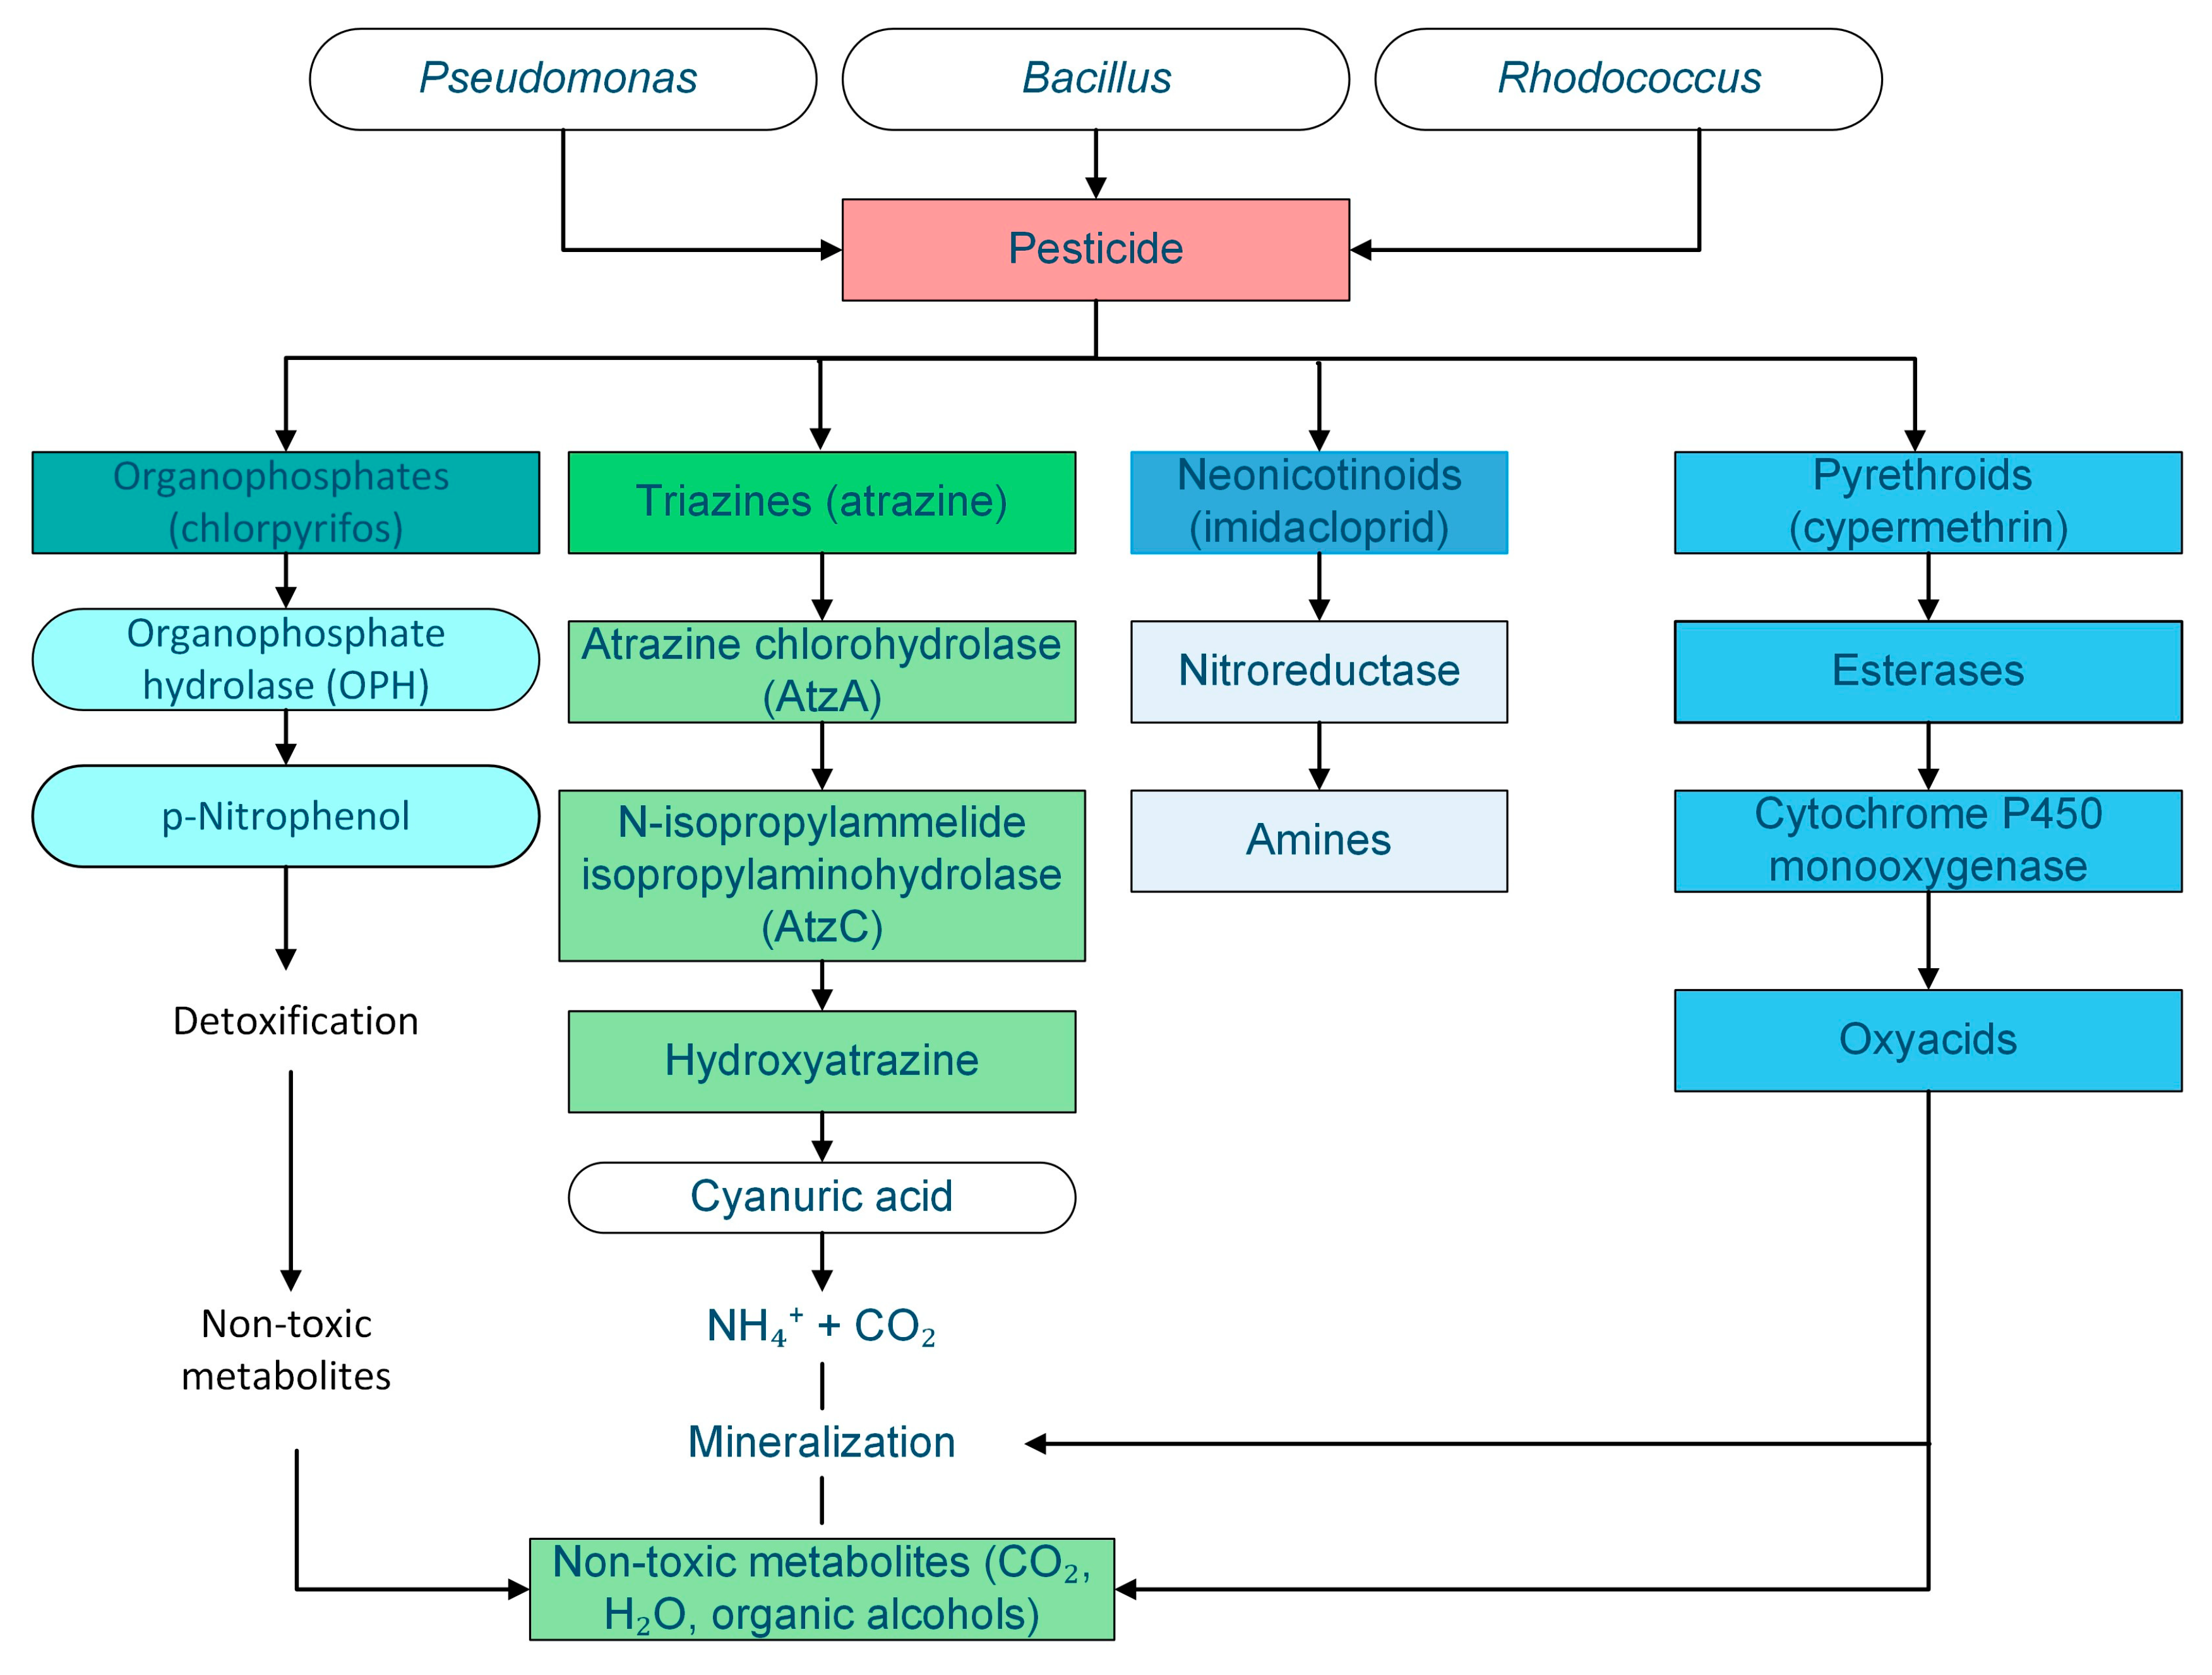
| Phosphotriesterases/Organophosphorus hydrolases (PTE/OPH) | Organophosphates (e.g., chlorpyrifos, diazinon, methyl parathion) | Hydrolysis of P-O bonds | Pseudomonas Roseomonas, Sphingobium, Bacillus, Arthrobacter | [10,98,99,104,106] |
| Carboxylesterases/Esterases | Carbamates, Pyrethroids | Ester hydrolysis, Ring opening | Bacillus, Pseudomonas, Rhodococcus, Acinetobacter, Stenotrophomonas | [21,44,45,64] |
| Nitroreductases | Neonicotinoids, Diphenyl ethers, Nitroaromatic | Nitroreduction, Demethylation, Nitroreduction | Bacillus, Rhodococcus Arthrobacter, Enterobacter, Klebsiella | [73,107,108] |
| Cytochrome P450 Monooxygenases/ Other Monooxygenases | Neonicotinoids, Organochlorines, Pyrethroids, Fungicides | Oxidative degradation (hydroxylation, dealkylation, N-oxidation) | Sphingomonas, Alcaligenes, Pseudomonas, Bacillus, Streptomyces | [95,96,97,109] |
| Amidases/Hydrolases | Carbamates, Triazines | Amide bond cleavage | Arthrobacter, Pseudomonas, Burkholderia, Variovorax, Paenarthrobacter | [23,43,61,110] |
| Oxidases (e.g., Laccases, Peroxidases, Multicopper oxidases) | Recalcitrant Pesticides, Aromatics, Dyes | Oxidation of aromatic rings, radical-mediated reactions | Pseudomonas, Ochrobactrum, Bacillus, Azospirillum, Streptomyces | [111,112,113,114,115] |
| Strategy | Description | Mechanism | Advantages | Limitation | Degradation Yield (%) | Time Duration | Examples | Sources |
|---|---|---|---|---|---|---|---|---|
| Natural Attenuation | Relies on indigenous microbes for passive degradation | Hydrolysis and oxidation by native enzymes | Cost-effective, minimal ecological disruption | Slow rates, incomplete mineralization (varies with soil conditions) | 30–60% | 30–90 days | Chlorpyrifos and endosulfan attenuation | [12,13,171,172,173] |
| Bioaugmentation | Introduces specific degraders to accelerate processes, using isolates or carrier materials | Esterase-mediated hydrolysis, nitroreduction | Targets specific contaminants, accelerates degradation | Strain survival, competition with natives, cost of inoculation | 70–95% chlorpyrifos & pyrethroids | 10–30 days | Bacillus sp. for chlorpyrifos, Rhodococcus pyridinivorans Y6 for pyrethroids | [60,67,80,174] |
| Synthetic Microbial Consortia | Engineered combinations of strains for synergistic degradation, regulated by quorum sensing | Complementary enzymatic pathways (e.g., esterases, oxidases) via quorum sensing | Synergistic efficiency, adaptable to multi-contaminants | Complex engineering, regulatory hurdles (e.g., safety assessments) | >90% mineralization | 7–21 days | Pseudomonas and Bacillus consortia | [15,21,87,135,175,176,177] |
| Field-Scale (biobed/biomixture) Applications | Large-scale deployment of consortia and amendments | Enhanced degradation with straw–peat–soil or composted organic substrates/ biochar and consortia | Scalable, high efficiency | Requires monitoring, site-specific | 50–100% dissipation across multiple pesticide classes | 30–120 days depending on climate and substrate | Biobeds for chlorpyrifos; biochar for atrazine & Chlorpyrifos | [178,179,180,181,182,183,184,185,186,187] |
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content. |
© 2025 by the authors. Licensee MDPI, Basel, Switzerland. This article is an open access article distributed under the terms and conditions of the Creative Commons Attribution (CC BY) license (https://creativecommons.org/licenses/by/4.0/).
Share and Cite
Dhakal, G.; Thapa Magar, S.; Fujino, T. Pesticide Degradation by Soil Bacteria: Mechanisms, Bioremediation Strategies, and Implications for Sustainable Agriculture. Environments 2025, 12, 492. https://doi.org/10.3390/environments12120492
Dhakal G, Thapa Magar S, Fujino T. Pesticide Degradation by Soil Bacteria: Mechanisms, Bioremediation Strategies, and Implications for Sustainable Agriculture. Environments. 2025; 12(12):492. https://doi.org/10.3390/environments12120492
Chicago/Turabian StyleDhakal, Gyanendra, Srijana Thapa Magar, and Takeshi Fujino. 2025. "Pesticide Degradation by Soil Bacteria: Mechanisms, Bioremediation Strategies, and Implications for Sustainable Agriculture" Environments 12, no. 12: 492. https://doi.org/10.3390/environments12120492
APA StyleDhakal, G., Thapa Magar, S., & Fujino, T. (2025). Pesticide Degradation by Soil Bacteria: Mechanisms, Bioremediation Strategies, and Implications for Sustainable Agriculture. Environments, 12(12), 492. https://doi.org/10.3390/environments12120492


