Article

Tributary-to-Mainstream Aquatic Macroinvertebrate Discontinuities in the Colorado River, Southwestern USA


by
Lawrence E. Stevens
1,*,
Joseph H. Holway
1 and
Craig Ellsworth
2
1
Spring Stewardship Institute, 414 North Humphreys Street, Flagstaff, AZ 86001, USA
2
Western Area Power Administration, Salt Lake City, UT 84111, USA
*
Author to whom correspondence should be addressed.
Water 2026, 18(3), 395; https://doi.org/10.3390/w18030395
Submission received: 8 December 2025 / Revised: 22 January 2026 / Accepted: 29 January 2026 / Published: 3 February 2026
(This article belongs to the Special Issue Freshwater Ecosystems—Biodiversity and Protection: 2nd Edition)

Abstract

Tributary-to-mainstem discontinuities (TMDs) are understudied, but are likely common in river networks, arising from abrupt transitions in stream order and dominant ecological factors. We present a conceptual model of aquatic macroinvertebrate (AMI) TMD directionality and relative magnitude by contrasting the impacts of hydrography, geochemistry, and sediment transport on tributary-related channel-floor precipitate cementation and the mainstream embeddedness (burial) of channel-floor substrata in fine sediment. We test that model using AMI assemblage density/m2, species richness/sample, and diversity data from 24 tributaries confluent with the regulated Colorado River in Grand Canyon through pairwise and multivariate analyses of long-term discharge records and substrate and water-quality data in three habitats: tributaries, their confluences, and adjacent mainstream habitats. Mean AMI density decreased 2.7-fold from low to high cementation, 6.1-fold from low-to-high embeddedness, and 136.0-fold across combined gradients. We also analyzed pre-dam aquatic insect literature, finding that TMDs were naturally common in Glen Canyon upstream but were more strongly tributary-positive (discontinuity magnitude, Dmag = 0.62 in pre-dam Glen Canyon) compared to tributaries in the post-dam Grand Canyon (Dmag = 0.31). We conclude that, depending on Dmag directionality, tributary confluences can function as hotspots or barriers to AMI assemblage development. Our results demonstrate that TMDs are and were common in the contemporary regulated and natural unregulated Colorado River corridor, and we expand the concept of biotic discontinuity to improve understanding of fluvial ecosystem ecology and constraints on river and dam management.

1. Introduction

Physical fluvial ecosystem discontinuities are abrupt transitions in stream ecosystems arising from, for example, impoundment, the intersection of the mainstream channel with different parent rock stratigraphy, or a tributary with different hydrography or water quality, any of which can create a reach boundary (Figure 1); see, e.g., [1,2]. Ward and Stanford’s [3] serial discontinuity model was originally conceived as a stepped recovery of regulated rivers through downstream tributary flow and water-quality contributions, and it was framed in the context of the river continuum concept [4]. However, more recent models emphasize the importance of channel segmentation, with reach boundaries defined by changes in channel geomorphology, hydrography, sediment transport, and water quality that affect riverine biota; see, e.g., [5,6,7,8,9,10].
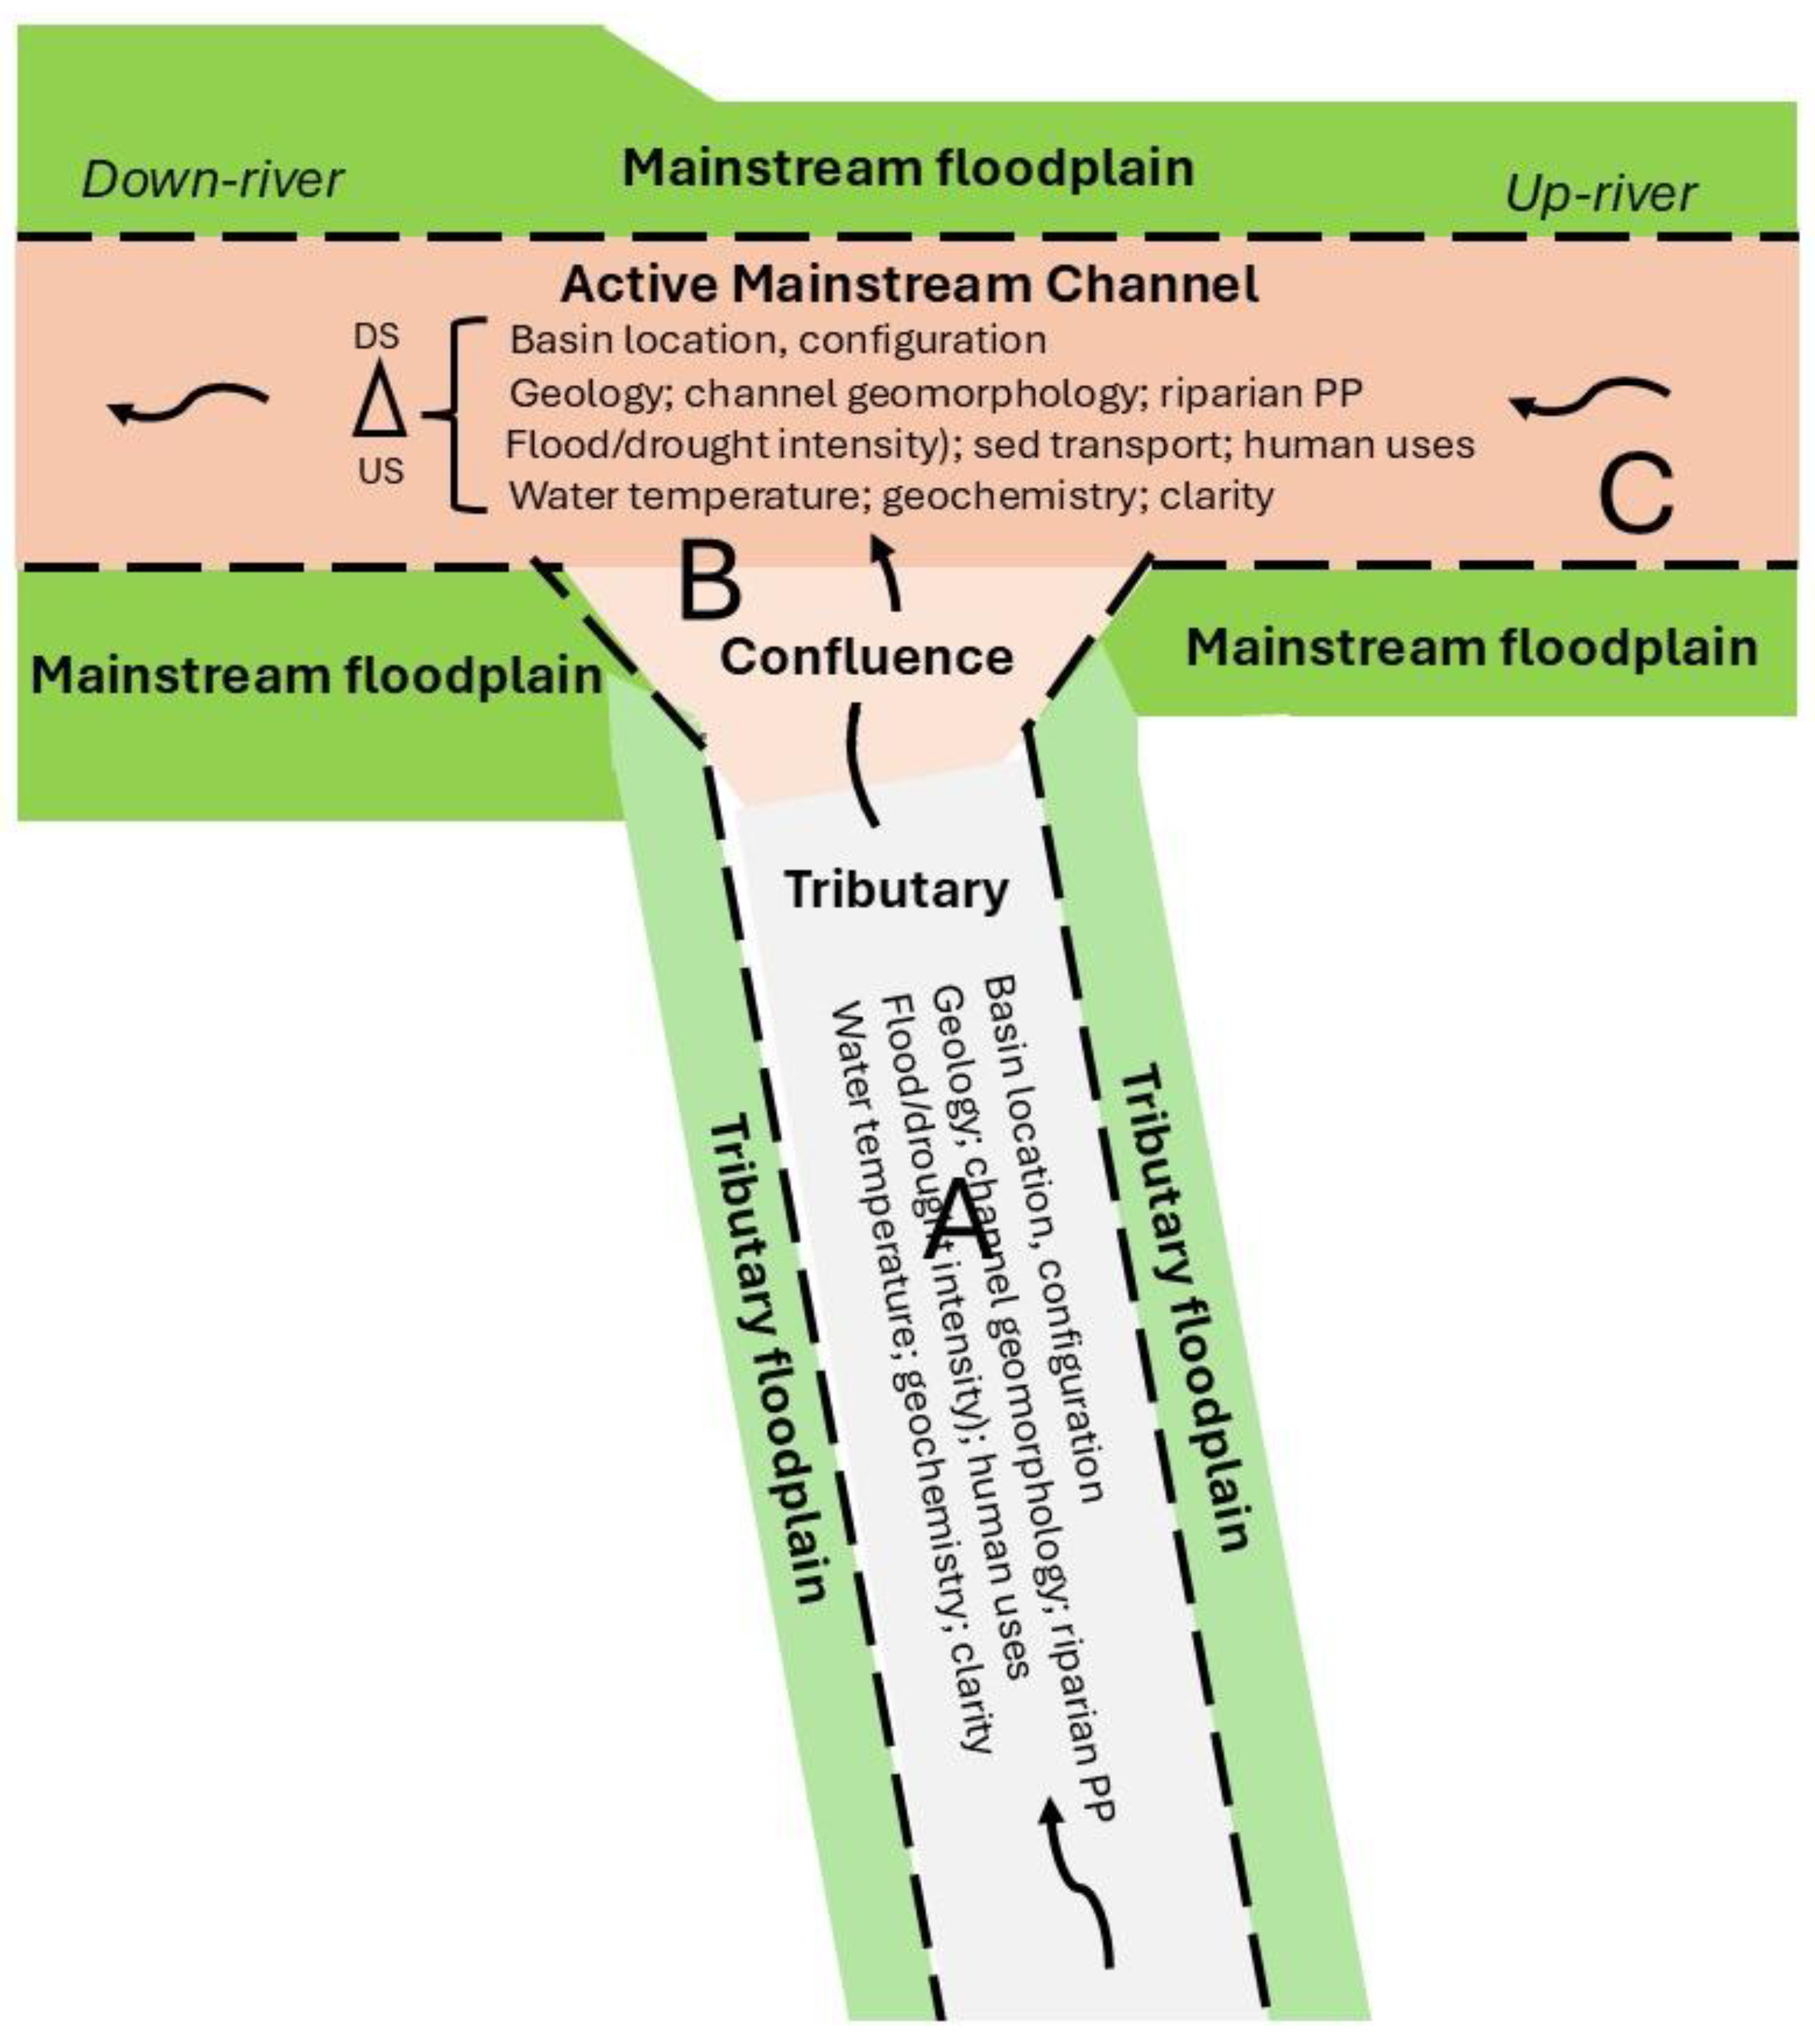
Tributary-to-mainstem discontinuities (TMDs) of aquatic macroinvertebrate (AMI) assemblages are not widely reported or explained but are likely common, arising from abrupt transitions in physical characteristics and processes between the two streams and their shared ecotonal confluence (mouth) habitat (Figure 1) [5,7,8]—reviewed in [9]. Following Dye [9], we posit that the direction and magnitude of AMI TMDs is related, either negatively or positively, to the extent of difference in hydrography, water quality (i.e., temperature, geochemistry), and/or sediment transport between the ecological characteristics of the tributary and the mainstream (Figure 1). A small, physically distinctive tributary (e.g., a geochemically precipitating or geothermal stream) is likely to demonstrate a larger AMI discontinuity with the mainstream river to which it is confluent, whereas a tributary of any size with fluvial characteristics and processes similar to those of its mainstream should generate a minor or neutral discontinuity. AMI assemblage complexity is often related to the diversity of suitable substrate habitats and is reduced by the loss of interstitial benthic refugia through the embeddedness of firm substrata in fine sediment or by geochemical precipitation that cements channel-floor substrata. Pollution, changes in sediment loading, or the flow regulation of a tributary or its mainstream river can augment, neutralize, or reverse the natural magnitude and directionality of a TMD. The inclusion of TMDs in consideration of the ecology of both regulated and unregulated stream networks expands the applicability of Ward and Stanford’s [3] serial discontinuity concept to natural rivers, extends the influence of Junk et al.’s [10] flood-pulse disturbance impacts on benthic habitat quality, and supports Thorp and Delong’s [11] river productivity model.
To test the hypothesis that biotic TMDs are common phenomena controlled by the magnitude of physical differences between the tributary and its mainstream, we compared AMI assemblage structure, composition, and similarity in 24 perennial, nearly pristine Colorado River tributaries with those in the confluence zones (mouth areas influenced by both streams) and the regulated mainstream in Grand Canyon. Abrupt transitions in AMI assemblages in this system were previously reported by Hofknecht [12], Oberlin et al. [13], and Stevens et al. [2] at Grand Canyon tributary confluences, and multiple authors have confirmed low AMI richness in the mainstream [2,12,13,14,15,16,17,18,19,20]. Perennial tributaries in this system vary widely in catchment area, geomorphology, hydrography, sediment transport, water quality (i.e., temperature and geochemistry) [12,21,22,23,24,25,26,27,28], and channel characteristics [1]. In contrast, the mainstream Colorado River has been regulated by Glen Canyon Dam since 1963, with stabilized discharge, variation in geochemistry, and year-round cool stenothermic water temperature [14,15,16,17,18,19,20]. Post-dam mainstream turbidity varies temporally and spatially in relation to large tributary contributions of fine sediment inputs, with occasionally prolonged periods of clearwater flow [15,21].
Oberlin et al. [13] proposed that catchment area was a primary factor influencing tributary AMI species richness in the Grand Canyon basin, and others have concluded that the depauperate mainstream condition was unnaturally related to thermal and daily flow variability due to impoundment [18,19,20]. We previously examined the TMD at Tapeats Creek, a cool, clearwater tributary in central Grand Canyon with water quality that closely matches the thermal and geochemical characteristics of the Colorado River released from Lake Powell through Glen Canyon Dam [2,15]. The profound reduction in AMI compositional diversity and density from that tributary to the mainstream was empirically and experimentally demonstrated to be related to the availability of interstitial space among firm substrata (gravel, cobble, boulder, woody debris) in the tributary channel as opposed to the embeddedness of benthic substrata in fine sand in the mainstream. Without the hyporheic interstitial space in gravel that characterized the tributary channels, the mainstream lacked the refugial benthic habitat needed by many AMI. However, additional data were needed to broaden our understanding of TMD distribution and dynamics in larger, smaller, and more chemically enriched tributaries.
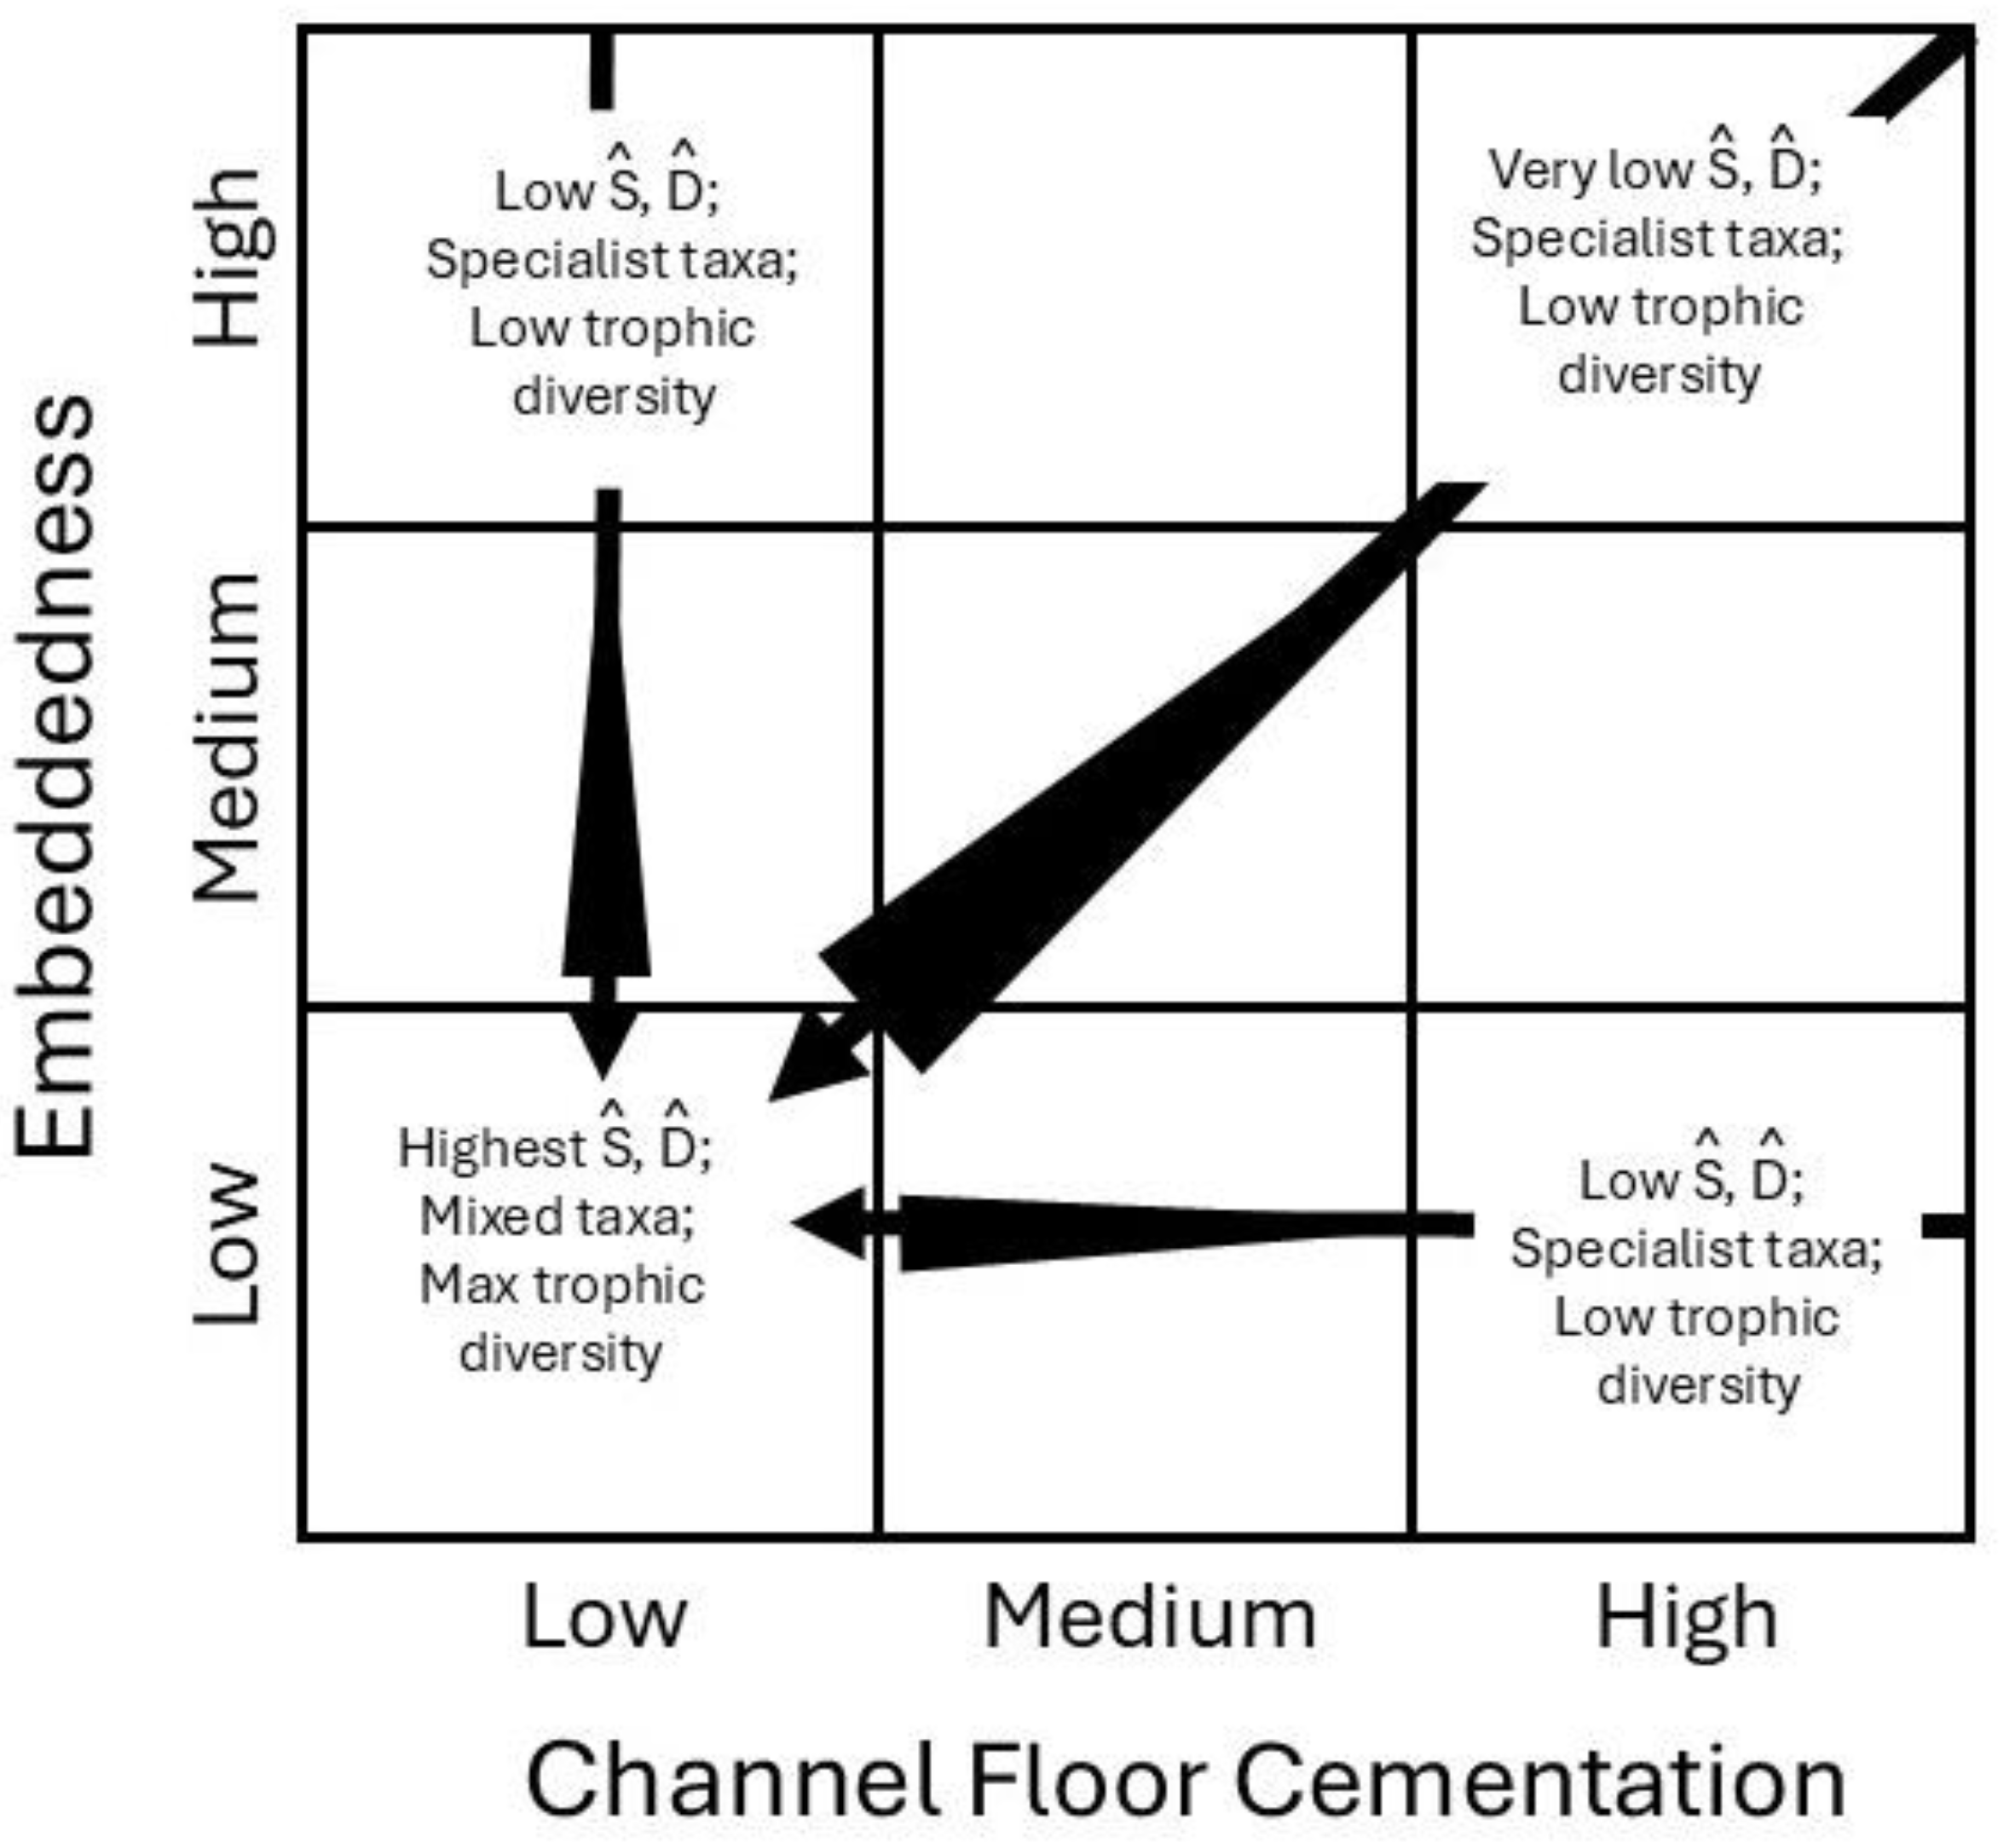
Here, we examine TMD distribution and directionality among a wide array of Colorado River tributaries in Glen and Grand Canyon, expanding the regional and temporal scope of our previous work. We specifically predicted that geochemical cementation of Colorado River tributary channel floors in geochemically-enriched streams, as well as mainstream deposition of fine sand, were both likely to reduce AMI species richness/sample and density/m2 (Figure 2). Tributary channel-floor cementation was expected to vary in relation to stream geochemistry and would be reduced in confluence zones by dilution or occasional turbulence due to variation in mainstream discharge. Sediment transport of fine sand was expected to embed firm substrata (rocks and coarse woody debris) in the mainstream, as well as in tributary mouths. Compounded influences of both cementation and embeddedness were expected to further reduce AMI assemblage composition, complexity, and function. We generated a metric to express the magnitude and direction of TMDs (Dmag), and we use it and empirical data to test the frequency, strength, and directionality of TMDs on AMI assemblages. To assess whether TMDs occurred in the Colorado River basin before impoundment, we compared our results to the historic pre-dam AMI assemblage data from tributaries, confluence zones, and the mainstream in the Glen Canyon basin upstream from Grand Canyon [29]. Our results indicate that TMDs were, and remain, common in the central Colorado River basin, supporting the proposed TMD conceptual model and providing insight into constraints on aquatic food base development in this, and likely many other natural and regulated river ecosystems.

2. Materials and Methods

2.1. Study Area

Catchment-scale channel physiognomy, sediment transport, and water quality in the 472 km long Colorado River between Glen Canyon Dam and Lake Mead, Arizona in Glen and Grand Canyons vary temporally and over distance among reaches and turbidity segments (Figure 3) [1,14,15,16,17,21,26,27,28]. Glen Canyon Dam is managed by the US Bureau of Reclamation for water delivery, hydropower production, and resource protection, as well as fine sediment retention for recreational river running, endangered fish, and indigenous tribal values, in particular [25]. Dam discharge varies seasonally within a normal range of 142–708 m3/s, but with (at the time of writing) a base flow of no less than 142 m3/s and a daily change of no more than 227 m3/s, resulting in a diel-stage fluctuation of approximately 0.5 m. Mainstream water temperature at the dam varies seasonally and interannually from 9 to 17 °C, warming over distance downstream in summer and cooling in winter. In contrast, the pre-dam river warmed to 29 °C during mid-summer and occasionally froze over during mid-winter [14,23,30]. Specific conductance of modern river water is typically 700–850 μS/cm2. The river corridor is managed by the US National Park Service, the Arizona Game and Fish Department, and the Navajo and Hualapai Tribes, with the latter two among at least six indigenous tribes with direct cultural affinity to the landscape [25].
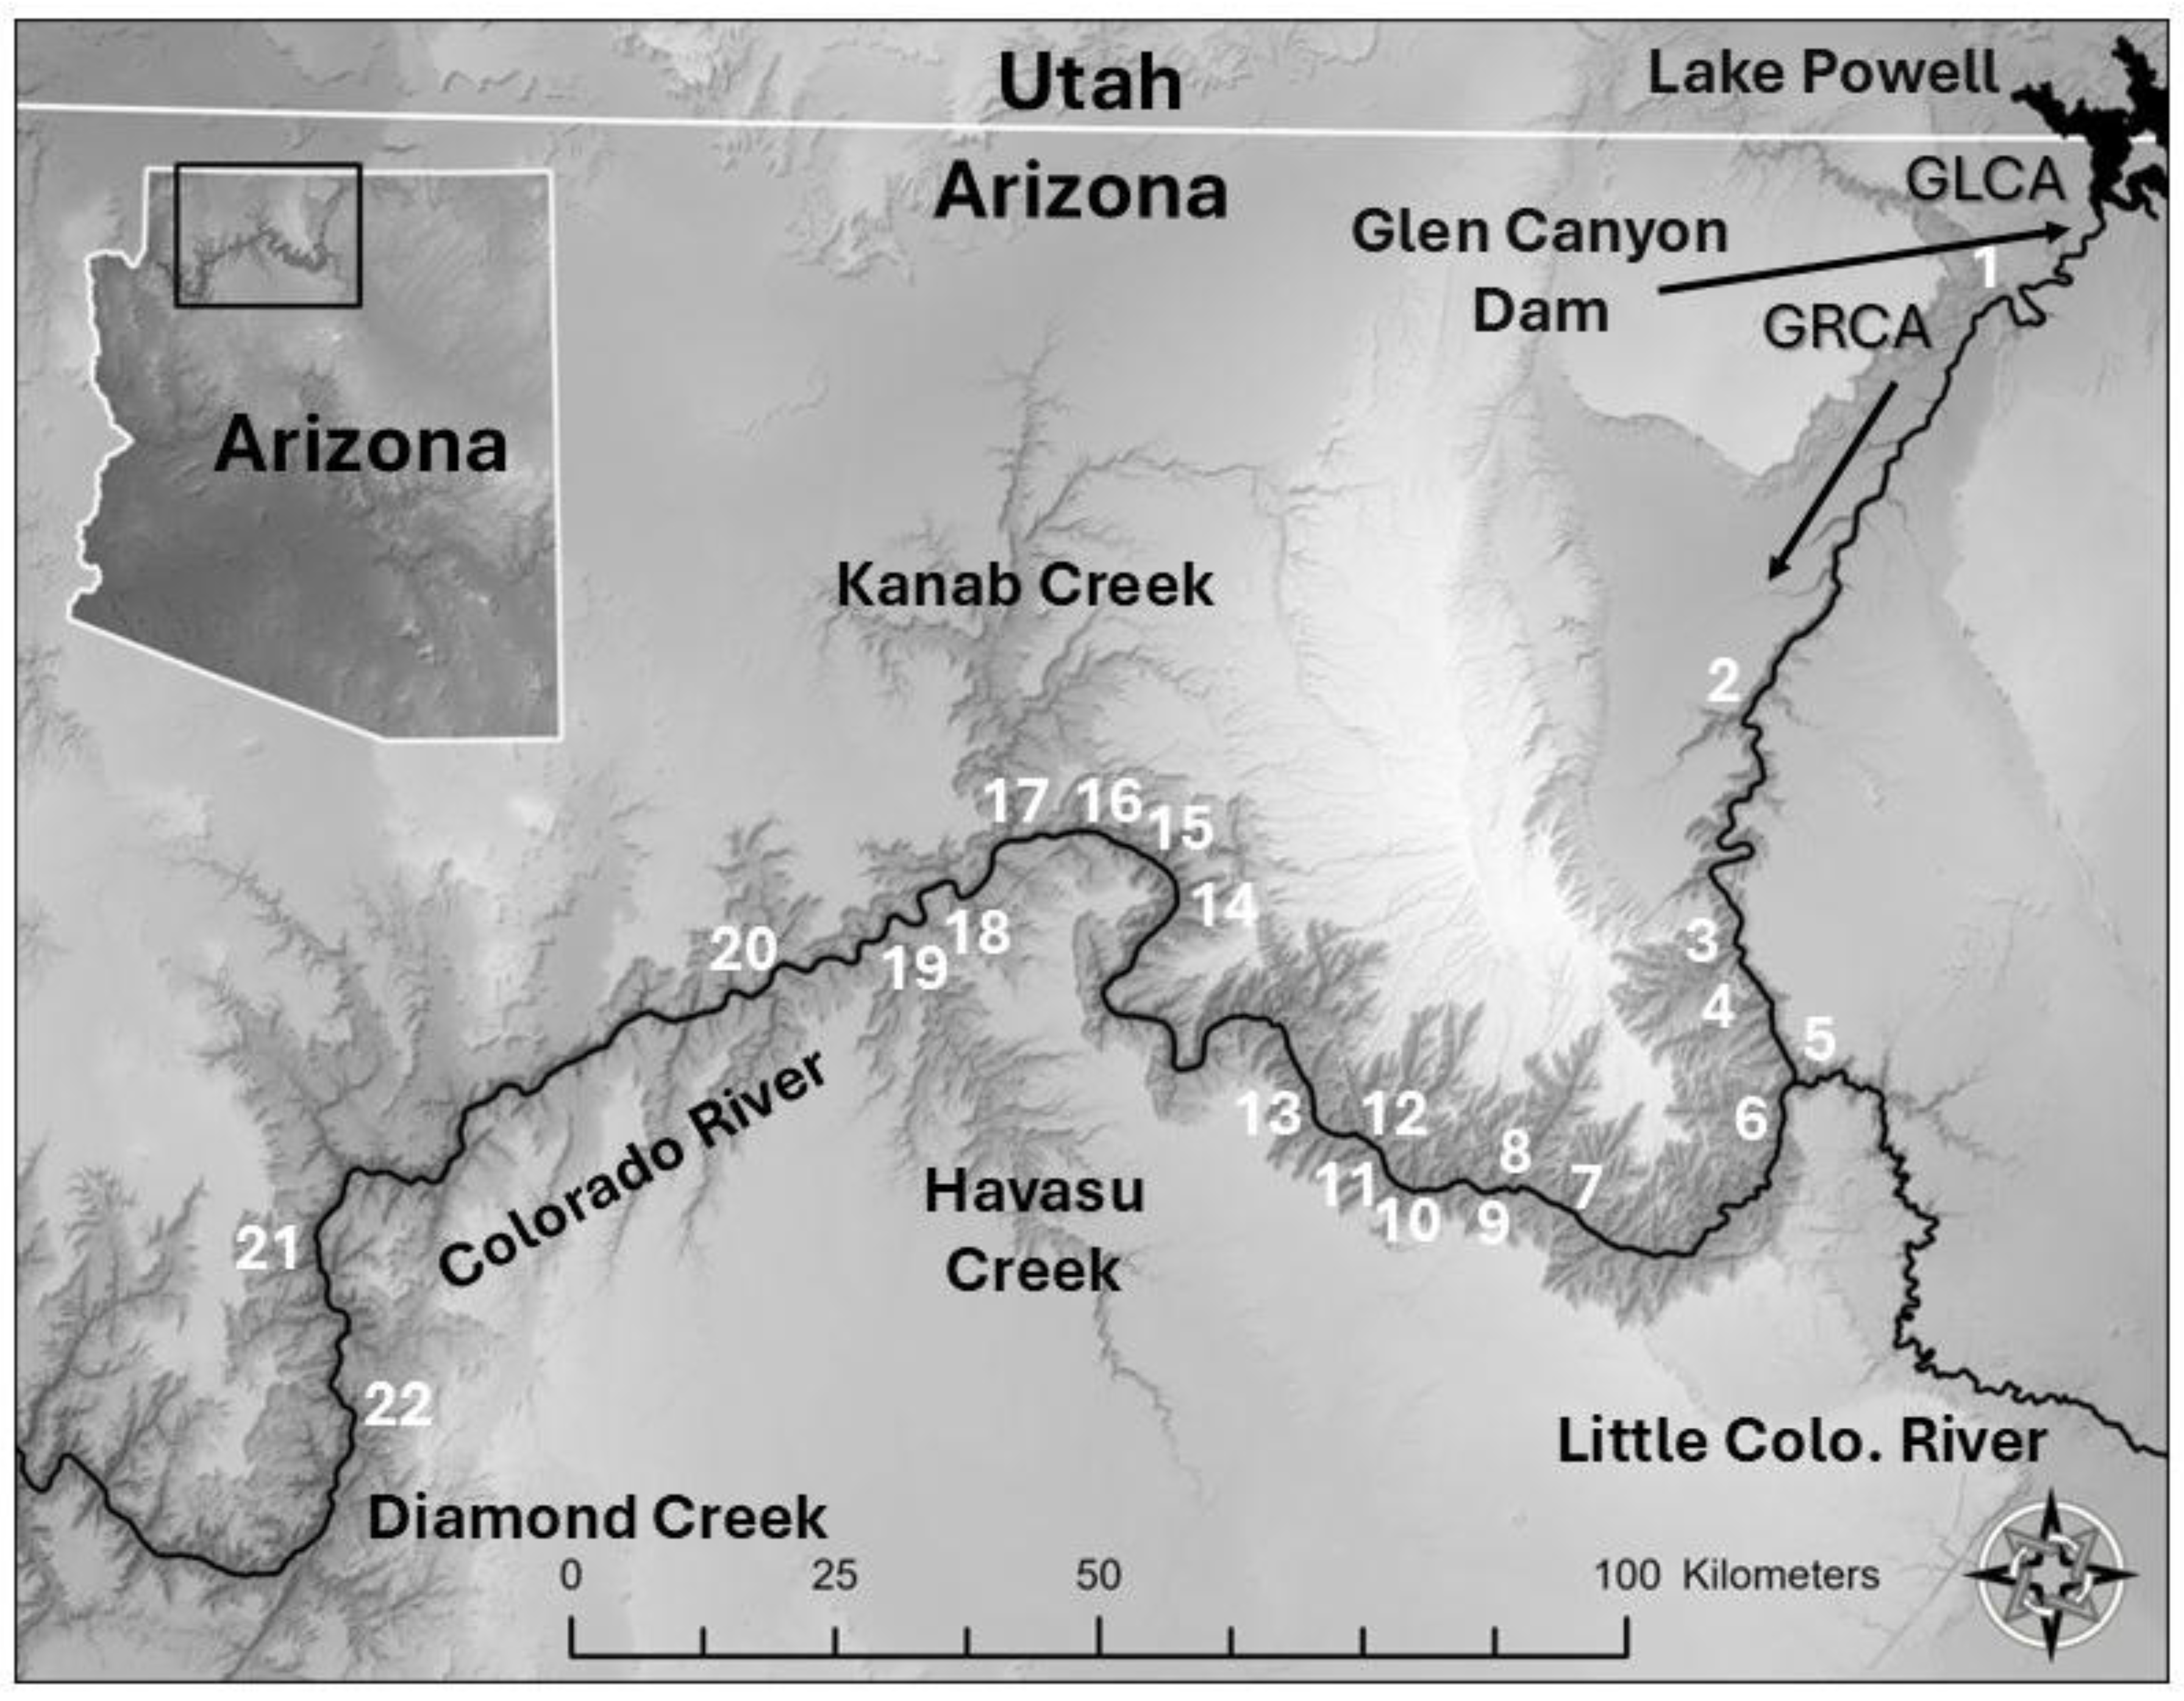
Figure 3. Map of the Colorado River in Glen Canyon National Recreation Area (GLCA) and Grand Canyon National Park (GRCA), Arizona. Sampling locations and numbers are listed in Table 1.
Water 18 00395 g003
The Colorado River receives flow from >50 perennial tributaries along its course through Glen and Grand Canyons, the surface catchments of which vary from less than 0.1 ha (e.g., Pumpkin Spring) to 69,000 km2 (i.e., the Little Colorado River). The larger tributary drainages extend far beyond the boundaries of the national park [13,17]. Tributary confluence zones are geomorphologically diverse, although most are tightly canyon-bound, although larger tributaries typically have low-gradient mouths. Precipitation in the region is bimodal, with winter storms and summer monsoons that generate runoff flooding, but the base flow of all tributaries in this system is derived from springs emerging from perched aquifers among the geologic strata for which Grand Canyon is renowned [17,31,32,33]. Tributary water temperature varies widely (9 °C to >35 °C) due to seasonal warming. No geothermal springs emerge in Grand Canyon, and the highly mineralized Pumpkin Spring (Rkm 341 downstream from Lees Ferry) is one of the few warm springs in the system. Baseflow geochemistry also varies widely [13,22]: specific conductance varying from 336 μS/cm2 at Vaseys Paradise to 33,767 μS/cm2 at Chuar Creek. Tributaries in central Grand Canyon, such as Bright Angel, Shinumo, Tapeats, and Deer Creeks, as well as Surprise Canyon in the lower Canyon are derived from karstic aquifers and are cool, clear water streams. Other tributaries, particularly those in the upper and lower Canyon are sourced from aquifers with longer residence time, with greater solute concentration, and waters that warm seasonally and/or actively precipitate travertine (e.g., the Little Colorado River, Havasu Creek).

2.2. Data Collection

L.E.S. and C.E. participated in a 16-day river trip through Grand Canyon from Lees Ferry to Diamond Creek with Grand Canyon Youth (GCY) during the pre-monsoon season (14–29 July 2023; Supplemental Information Table S1). With the assistance of GCY participants as citizen scientists, SSI staff sampled three habitats (where possible) in 17 tributaries: (1) the tributary above the mainstream 1275 m3/s stage (the zone not affected by recent dam operations); (2) the “inter-fluvial” tributary mouth habitat that is regularly inundated by daily–annual mainstream hydroelectric discharge variation; and (3) the mainstream not influenced by the tributary (across the river or upstream from the mouth; Figure 1). Additional observations were made at seven other tributaries during expeditions in May-June 2024 and September–October 2025, for a total of 24 tributaries compared in this analysis (Figure 3). Not all tributaries flowed to the mainstream, resulting in unequal totals of the three habitats sampled/site.
We measured or obtained data on variation in discharge and/or water quality from field measurements and the literature; see, e.g., [21,22,23,24]. Field tributary discharge was measured using a wading rod and SwofferTM flow meter (Federal Way, WA, USA) at 0.5 to 1.0 m intervals across the stream, where possible, with data integrated to estimate discharge. In tributaries with low discharge, flow was measured using timed flow capture methods. Field water quality was measured using a daily-calibrated Hanna Combo MeterTM (Woonsocket, RI, USA), including: temperature, pH, specific conductance, total dissolved solid concentration). Benthic sample depth, velocity, and sampled area were measured and substratum composition was visually estimated in each of the three samples/habitat as the percent cover of surficial fine (ooze, silt, sand) particles in relation to larger grain sizes in the sampled area. The sampled area was occasionally smaller where stream channels were small Table S2). Benthic cementation was visually estimated in each sample as low, medium, or high in extent.
The AMI assemblage was sampled using Hess samplers or dip nets (0.5 mm mesh), documenting benthic substrate composition and AMI density (number of individuals)/m2 and species richness/sample in each habitat. Sampling was conducted at haphazardly selected points in each habitat, working in an upstream direction. An area of 0.09 m2 of the channel floor was vigorously disturbed upstream from the sampler for one minute and AMIs that washed into the net were collected in 80% EtOH or tallied in the field. Three or more samples were collected in each microhabitat. Specimens were sorted to morpho-species to order or lower taxonomic level based on Merritt et al. [34].

2.3. Analyses

Hydrogeology: Drainage basin area data were compiled from Melis et al. [27], Webb et al. [28], and US Geological Survey online sources. Hydrology data were imported from USGS Water Data for The Nation using the R dataRetrieval package version 4.2.2. (31 October 2024). We used the R Discharge package to perform a Discrete Fast Fourier Transformation (DFFT). DFFT is used on hydrology time-series data to identify dominant periodic patterns, such as seasonal cycles or storm events [35], to characterize hydrologic regimes by revealing how different frequencies contribute to system behavior, including flashiness or long-term trends and subsequent effects on downstream ecology [35,36,37]. This analysis supports comparison across basins, the detection of hydrographic change over time, and the simplification of complex data for use in analyses of, in our case, determining the effects of hydrologic regime characteristics on AMI composition.
We characterized hydrographic regime characteristics using six drivers: range in net annual anomaly (rNAA), minimum highest spectral anomaly magnitude (minHSAM), maximum highest spectral anomaly magnitude (maxHSAM), range in highest spectral anomaly magnitude (rHSAM), inter-flood interval (IFI), and inter-drought interval (IFI). rNAA captures interannual variation in discharge, whereby a low value, typical of the dam-controlled Colorado River through Grand Canyon represents relatively consistent discharge volume year after year. Alternatively, a large rNAA value represents high interannual variation, typical of many Grand Canyon tributaries known for highly variable and intense flood events related to highly localized weather events; see, e.g., [24,26]. HSAM flood magnitude was analyzed in relation to seasonality. The larger the HSAM value, the larger the flood event in relation to the long-term seasonal signal. Therefore, minHSAM, maxHSAM, and rHSAM all characterize flood events as they relate to the long-term seasonal signal. Lastly IFI refers to the average number of days between flood events, while IDI is the average number of days between low-flow events. These metrics capture the frequency and timing of hydrologic extremes for inter-basin comparisons, the detection of temporal change, and simplify complex data to facilitate the understanding of flow regime influences on ecological processes, such as local AMI habitat structure.
We analyzed long-term hydrologic variability among seven sites using two complementary metrics: net annual anomaly (NAA) range and highest spectral anomaly magnitude (HSAM). The NAA range quantifies interannual variation, where positive values indicate wetter-than-average years and negative values indicate drier-than-average years. HSAM captures the magnitude of extreme flood events within each drainage.
Biota: AMI samples collected in 2023 were returned to the laboratory for sorting, identification, and enumeration under 10-X magnification, while AMI from subsequent samples were tallied in the field. The number of Ephemeroptera, Plecoptera, and Trichoptera (EPT) individuals in each sample was summed and used as an assemblage metric, as recommended by the US Environmental Protection Agency e.g., [38]. While the AMI assemblage in the Colorado River downstream from Glen Canyon Dam is highly altered and a management concern [25], most Grand Canyon tributaries are in nearly pristine condition [17]. However, many tributaries naturally support few EPT [13]; thus, the EPT metric should not be misconstrued as a metric of stream ecosystem integrity in this landscape.
Analyses of AMI composition and structure were visually depicted and statistically analyzed using pairwise comparisons in anticipation of the R-based multivariate characterization of assemblage structure to physical variables. General and non-linear regression analyses were used to relate AMI species richness/sample and density/m2. Canonical correspondence analysis (CCA) was employed to explore the relationships between benthic macroinvertebrate communities and both substrate and hydrologic variables. CCA is a widely used constrained ordination technique in ecological studies that is particularly well-suited for species–environment data, as it directly relates variation in community composition to measured environmental gradients. It assumes unimodal species responses and is effective when the goal is to identify which environmental factors most strongly influence species distributions. This method was chosen because it allowed for simultaneous analysis of multiple environmental variables while accounting for their combined effects on biological assemblage complexity. To meet the assumptions of normality and linearity, species density data were Hellinger-transformed prior to analysis. Within the environmental variables, we calculated Pearson correlation coefficients, and any variables with r > 0.9 were excluded from subsequent analyses to avoid multicollinearity. Analyses were conducted in R using the vegan package, and the significance of the environmental variables was evaluated using a Monte Carlo permutation test based on an ANOVA-like framework. Two separate CCAs were conducted. The first CCA evaluated the influence of hydrologic variables; however, due to the limited availability of long-term hydrologic data, only a subset of sites with sufficient flow records were included in this analysis. The second CCA focused on assessing relationships between AMI assemblages and benthic substrate characteristics across all sampled sites.
To quantify the magnitude and directionality of AMI assemblage discontinuity between a tributary and the mainstream, we developed a simple magnitude of discontinuity metric (Dmag) using species presence–absence data through the following formula:
Dmag i = (ST iSM i)/(ST i + SM i + SC i)
where ST i is the number of species unique to tributary i; SM i is the number for the mainstream; and SC i is the sum of richness of species common to both the tributary and the adjacent mainstream habitats at that site. Values of Dmag vary from −1.0, when there is a high richness of unique species in the mainstream and none in the tributary and no AMI species common to both habitats, to 1.0, when there is a high richness of unique species in the tributary but none in the mainstream and with no species in common (Table S2). For example, if there are 19 unique mainstream AMI species, 1 unique tributary species, and 5 species in common to both habitats, Dmag = −0.72, indicating a relatively large discontinuity with an enriched mainstream and depauperate tributary assemblage. If the tributary and the mainstream each have the same number of unique species in common, Dmag = 0.0 (no discontinuity, equivalent composition), no matter how many other species occur in the system. If a tributary has 19 unique species and the mainstream has just 1 unique species, and 5 other species in common, Dmag = 0.72, indicating a relatively large discontinuity with an enriched tributary but a depauperate mainstream assemblage.
In the case of the Tapeats Creek study mentioned above [2], an average of 4.8 species/sample were detected in the tributary samples (n = 36), while 1.0 species/sample were detected on average in the mainstream (n = 30), with no species in common. These data produced an average Dmag score of 0.66, indicating a large TMD with an enriched tributary assemblage and a depauperate mainstream condition. Notably, Dmag increased slightly to 0.68 in the unembedded, tumbling water at the downstream confluence channel at the Tapeats Creek mouth, but was lower (0.57) in the upstream runout confluence channel, which was a low-velocity habitat more fully embedded in mainstream-deposited fine sand. Those results suggest that intermediate disturbance dynamics [39,40,41] may play a role in AMI assemblage structure at some tributary confluences. Although more complex directional and similarity scoring using multivariate eigenvalues can be created, the Dmag metric presented here and based on simple presence–absence species richness data is sufficient for the purposes of discerning differences in the magnitude and directionality of TMDs among tributary confluences within and among mainstream rivers.
Disappointingly few data are available on the AMI fauna of the Colorado River in Grand Canyon prior to impoundment by Glen Canyon Dam in 1963 [2,14]. To better understand whether TMDs occurred naturally in the Colorado River, we reviewed Woodbury’s 1959 data on aquatic insects in the 290 km long Glen Canyon basin upstream from Grand Canyon [29], which was subsequently inundated under Lake Powell reservoir. His data did not allow for paired tributary-to-mainstream comparisons (and many zero samples from the river were not recorded). Therefore, we calculated only the basin-wide Dmag score using the presence of aquatic insect species reported for tributary, confluence, and mainstream habitats. Although focused just on aquatic insects, these pre-dam Glen Canyon data provided insight into the frequency of TMDs in the river prior to impoundment. By virtue of the sand-dominated mainstream conditions that prevailed in Glen Canyon prior to impoundment [14,21,25], his results likely reflect the frequency of occurrence of TMDs downstream in the pre-dam Colorado River corridor in Grand Canyon.

3. Results

3.1. Overview

Although the Colorado River mainstream in Grand Canyon is notoriously depauperate of AMI taxa [2,13,14,15,16,17], the 24 tributaries varied greatly in AMI composition, structure, and function, as well as in physical hydrography and water quality, fluvial geomorphology, and benthic substrate composition (Table 1 and Table 2; Table S1). While little evidence of recent flooding was observed at the sites sampled, the full suite of three habitats/tributary was compromised because the surface flow of Saddle Canyon and 167 Mile Spring did not reach the mainstream (no mouth habitat sampled); the mouth of Shinumo Creek sustains intensive visitor trampling and therefore was excluded from analyses; and the source of Pumpkin Spring lay below the 1275 m3/s stage, although the source area had not been recently affected by mainstream flows, and so data collected there were regarded as a tributary sample.

3.2. Hydrography and Physical Variables

Discharge among tributaries ranged from <0.1 L/s at Pumpkin Spring to a cross-sectional baseflow measurement of 6.18 m3/s at the Little Colorado River, varying episodically, seasonally, and interannually. The Paria River exhibited the highest hydrologic variability, with a 35-year record showing an NAA range of 136.57 and HSAM values ranging from 0.59 to 1.90, reflecting large flood magnitudes. Pump House Wash Spring, also with 16 years of data, displayed a similar NAA range (134.42) but had lower flood magnitudes (HSAM −0.18 to 0.56). Hermit Creek above Tonto Trail showed moderate variability (NAA range 73.55) and high flood magnitudes (HSAM 0.01–1.45). In contrast, larger streams, such as the regulated Colorado River at Lees Ferry and unregulated Havasu Creek above the confluence, exhibited lower NAA ranges (28.76 and 15.01, respectively) and relatively smaller flood magnitudes, indicating more stable flow regimes. Kanab Creek above the mouth had intermediate variability (NAA range 25.60; HSAM 0.16–0.54). Overall, these metrics highlight considerable differences in both interannual hydrologic variability and flood magnitude among the studied systems, with smaller tributaries and desert springs sustaining the greatest extremes.
The mainstream channel floor was dominated by open sand, with cobbles and boulders embedded in fine-grained sediments at most sites sampled (Table 1 and Table 2). Substrate composition varied widely among tributaries, with cool-water streams like Bright Angel, Tapeats, and Deer Creeks dominated by mixed sand, gravel, cobbles, and boulders, with little embeddedness and abundant interstitial refugial habitat. In contrast, the channel floors of lower gradient, geochemically enriched tributaries (e.g., the Paria and Little Colorado Rivers, Chuar and Havasu Creeks, Pumpkin Spring) were heavily cemented with carbonate precipitate and had little interstitial AMI refugial habitat. Tributary mouths were often intermediate between the channel substrate conditions of their tributaries and the fine sediment embeddedness created by varying stages of the mainstream (e.g., Kanab and Spring Creeks).
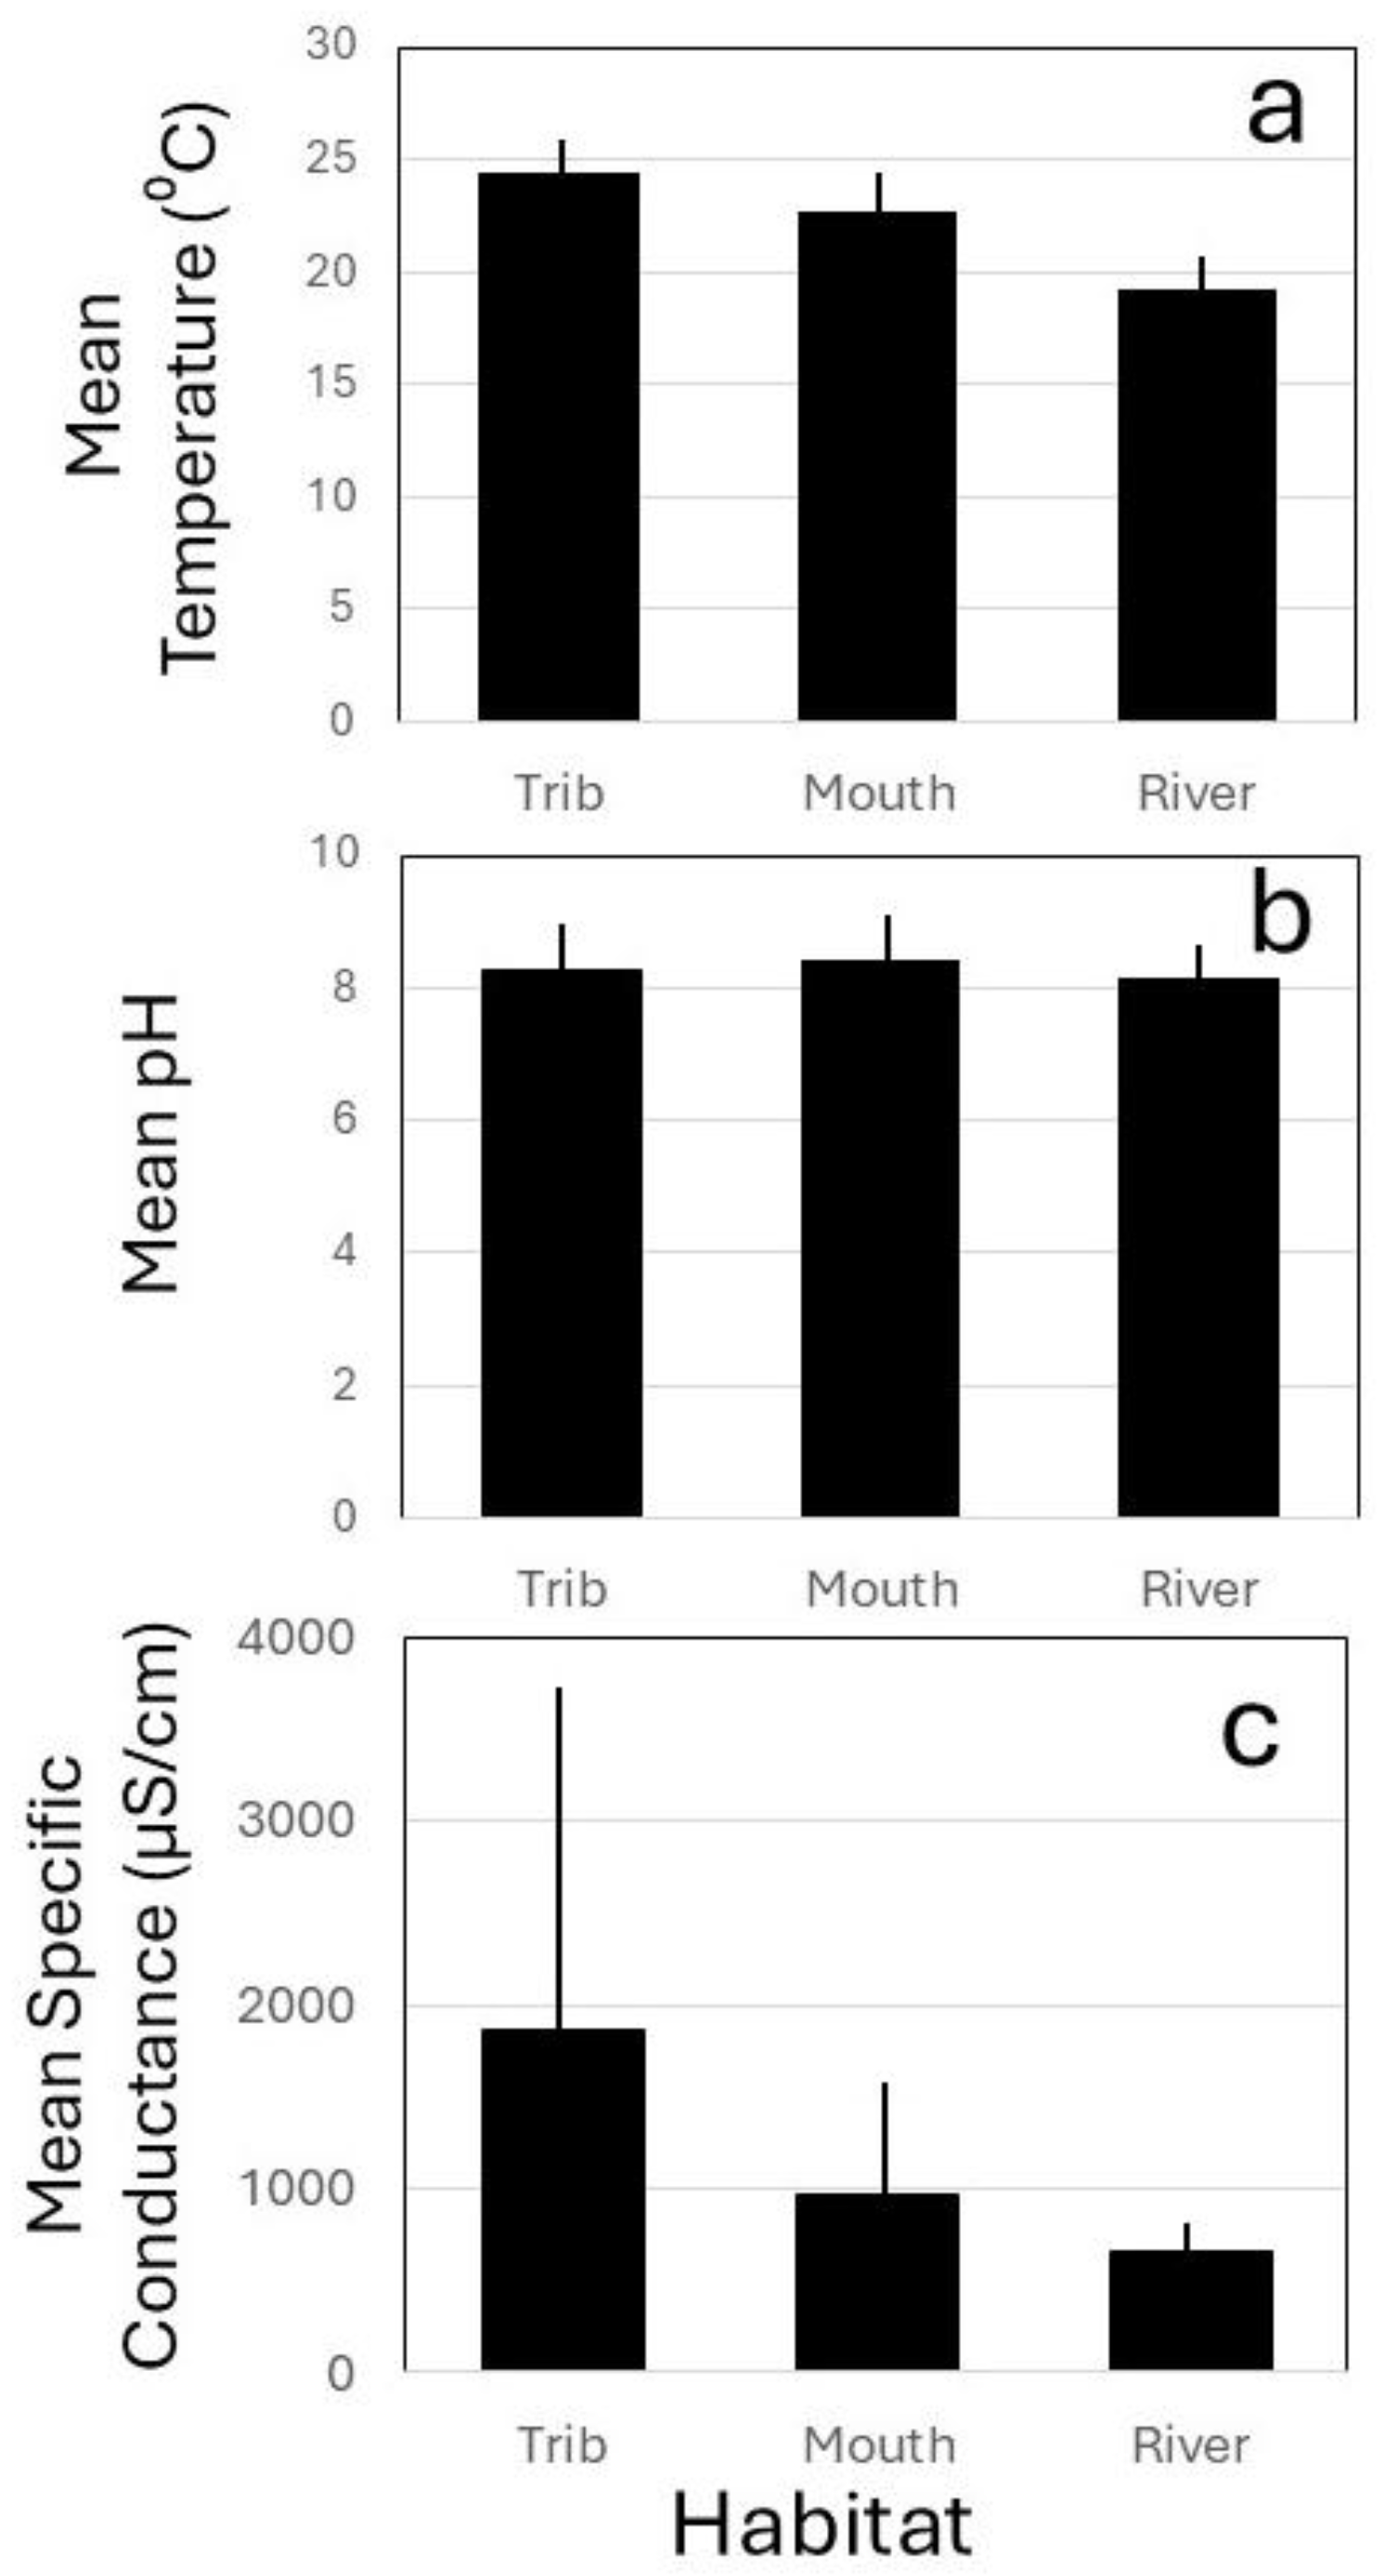
Water quality varied among habitats and in relation to tributary basin area and distance downstream through Grand Canyon (Table 1; Figure 4). Water temperature among all samples ranged from 13.5 °C (Hermit Creek) to 33.2 °C (Pumpkin Spring), with high tributary water temperature related to summertime air temperature in this desert landscape. We observed mid-summer water temperature in the Paria River of 38 °C, resulting in fish kills (L.E.S., unpublished data), and similarly warm summertime temperatures occur in Chuar and Kanab Creeks and Pumpkin Spring. In contrast, summertime temperature in tributary streams sourced by karstic springs rarely exceed 32 °C and are usually considerably cooler. Mainstream temperature increased over distance from Lees Ferry, ranging from 16.9 to 25.0 °C during our data collection, varying in relation to season (R2 = 0.171).
Tributary pH ranged from 6.30 (Pumpkin Spring) to 8.99 (Clear Creek), generally slightly to moderately basic and non-significantly decreasing over distance downstream (R2 = 0.056). Tributary pH was not related to log-transformed tributary basin area (R2 = 0.017). In contrast, mainstream pH increased slightly with distance downstream from Glen Canyon Dam (R2 = 0.308; Table 1; Figure 4b).
Tributary-related specific conductance (SC) ranged widely from 328 μS/cm2 (Vaseys Paradise) to 16,963 μS/cm2 (Chuar Creek; Table 1; Figure 4c), varying in a complex fashion over distance. Low values were associated with karstic groundwater emerging from springs on the Kaibab Plateau in central Grand Canyon, as well as Royal Arch Creek (south side of the river, mid-Canyon), and Surprise Canyon (north side, lower Canyon). In contrast, travertine-precipitating tributaries and those with flow derived from Precambrian or other aquifers often had high to very high values (e.g., the Paria and Little Colorado Rivers, Chuar and Kanab Creek, Pumpkin Spring). Log-transformed SC was weakly related to distance downstream (4th-order polynomial R2 = 0.333) and non-linearly related to log-transformed tributary basin area (3rd order polynomial R2 = 0.252), with the highest values at basin areas below 10 km2 and above 1000 km2 except for Chuar Creek, which was fed by a Precambrian-sourced spring 2 km upstream from its mouth.

3.3. AMI Distribution

We detected 11,361 AMI among 206 benthic samples, including at least 72 morpho-species in 47 families among 19 orders in eight classes in four phyla (Appendix A). We observed the following order of dominance among these taxa:
Insecta (Diptera > Ephemeroptera >> Coleoptera~Trichoptera >> Odonata >>
Hemiptera > Plecoptera) > Mollusca (Gastropoda > Bivalvia) >
Trombidiformes > Platyhelminthes > Tricladida > Oligochaeta >
Microcrustaceans.
In addition, we detected five orders of terrestrial insects among the samples but did not include them in assemblage or discontinuity calculations.
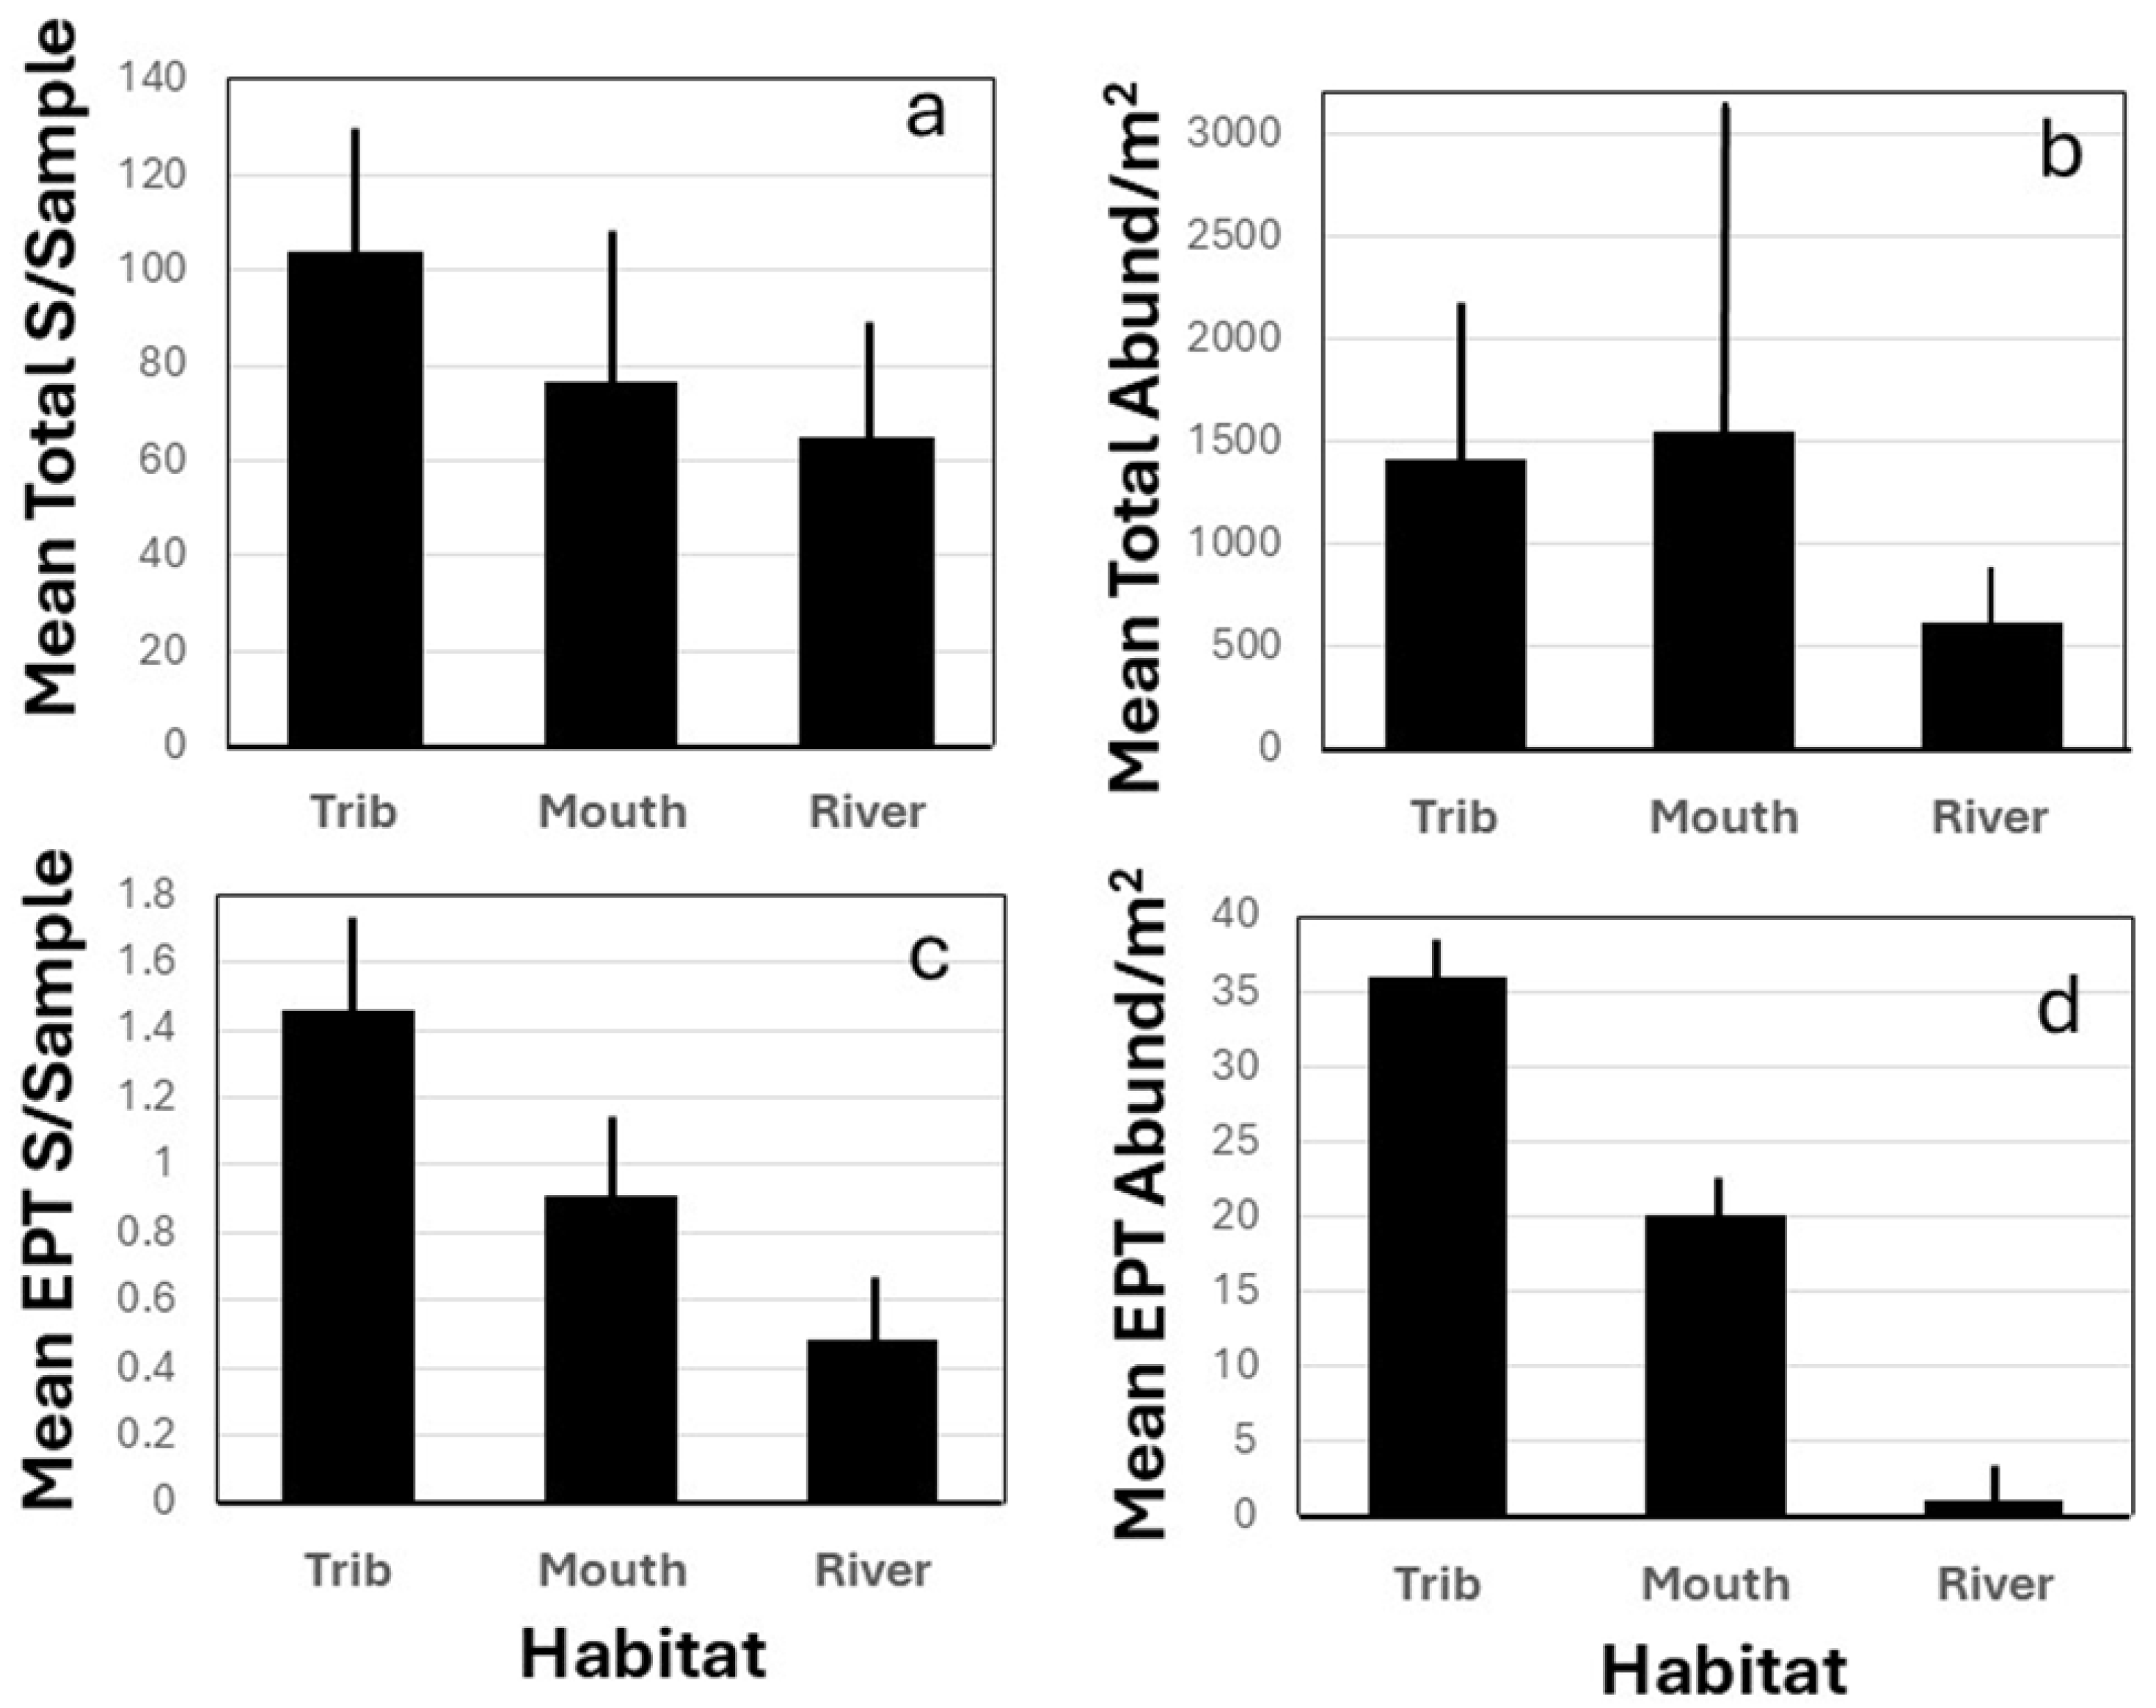
AMI mean species richness/sample and mean total density/m2, as well as those metrics for EPT taxa, decreased from the tributary through the confluence zones to the mainstream (Table 1; Figure 5). Species richness and density were greatest in the cooler-water tributaries emerging from karstic springs on the north side of the Colorado River (e.g., Vaseys Paradise, Clear, Bright Angel, Tapeats, and Deer Creeks) and were lower in travertine-depositing and other more solute-enriched tributaries (e.g., Little Colorado River, Pumpkin Spring). AMI assemblages in cool-water streams supported a wider array of feeding strategies and greater trophic complexity, with more predators (e.g., Corydalidae, Dytiscidae). Cool-water karstic-sourced AMI richness and density was higher, despite the presence of native and non-native fish in many of those tributary streams. In contrast, chemically enriched streams primarily supported grazing and ooze-dwelling taxa (Physidae snails, Chironomus midges, and other nematoceran flies).
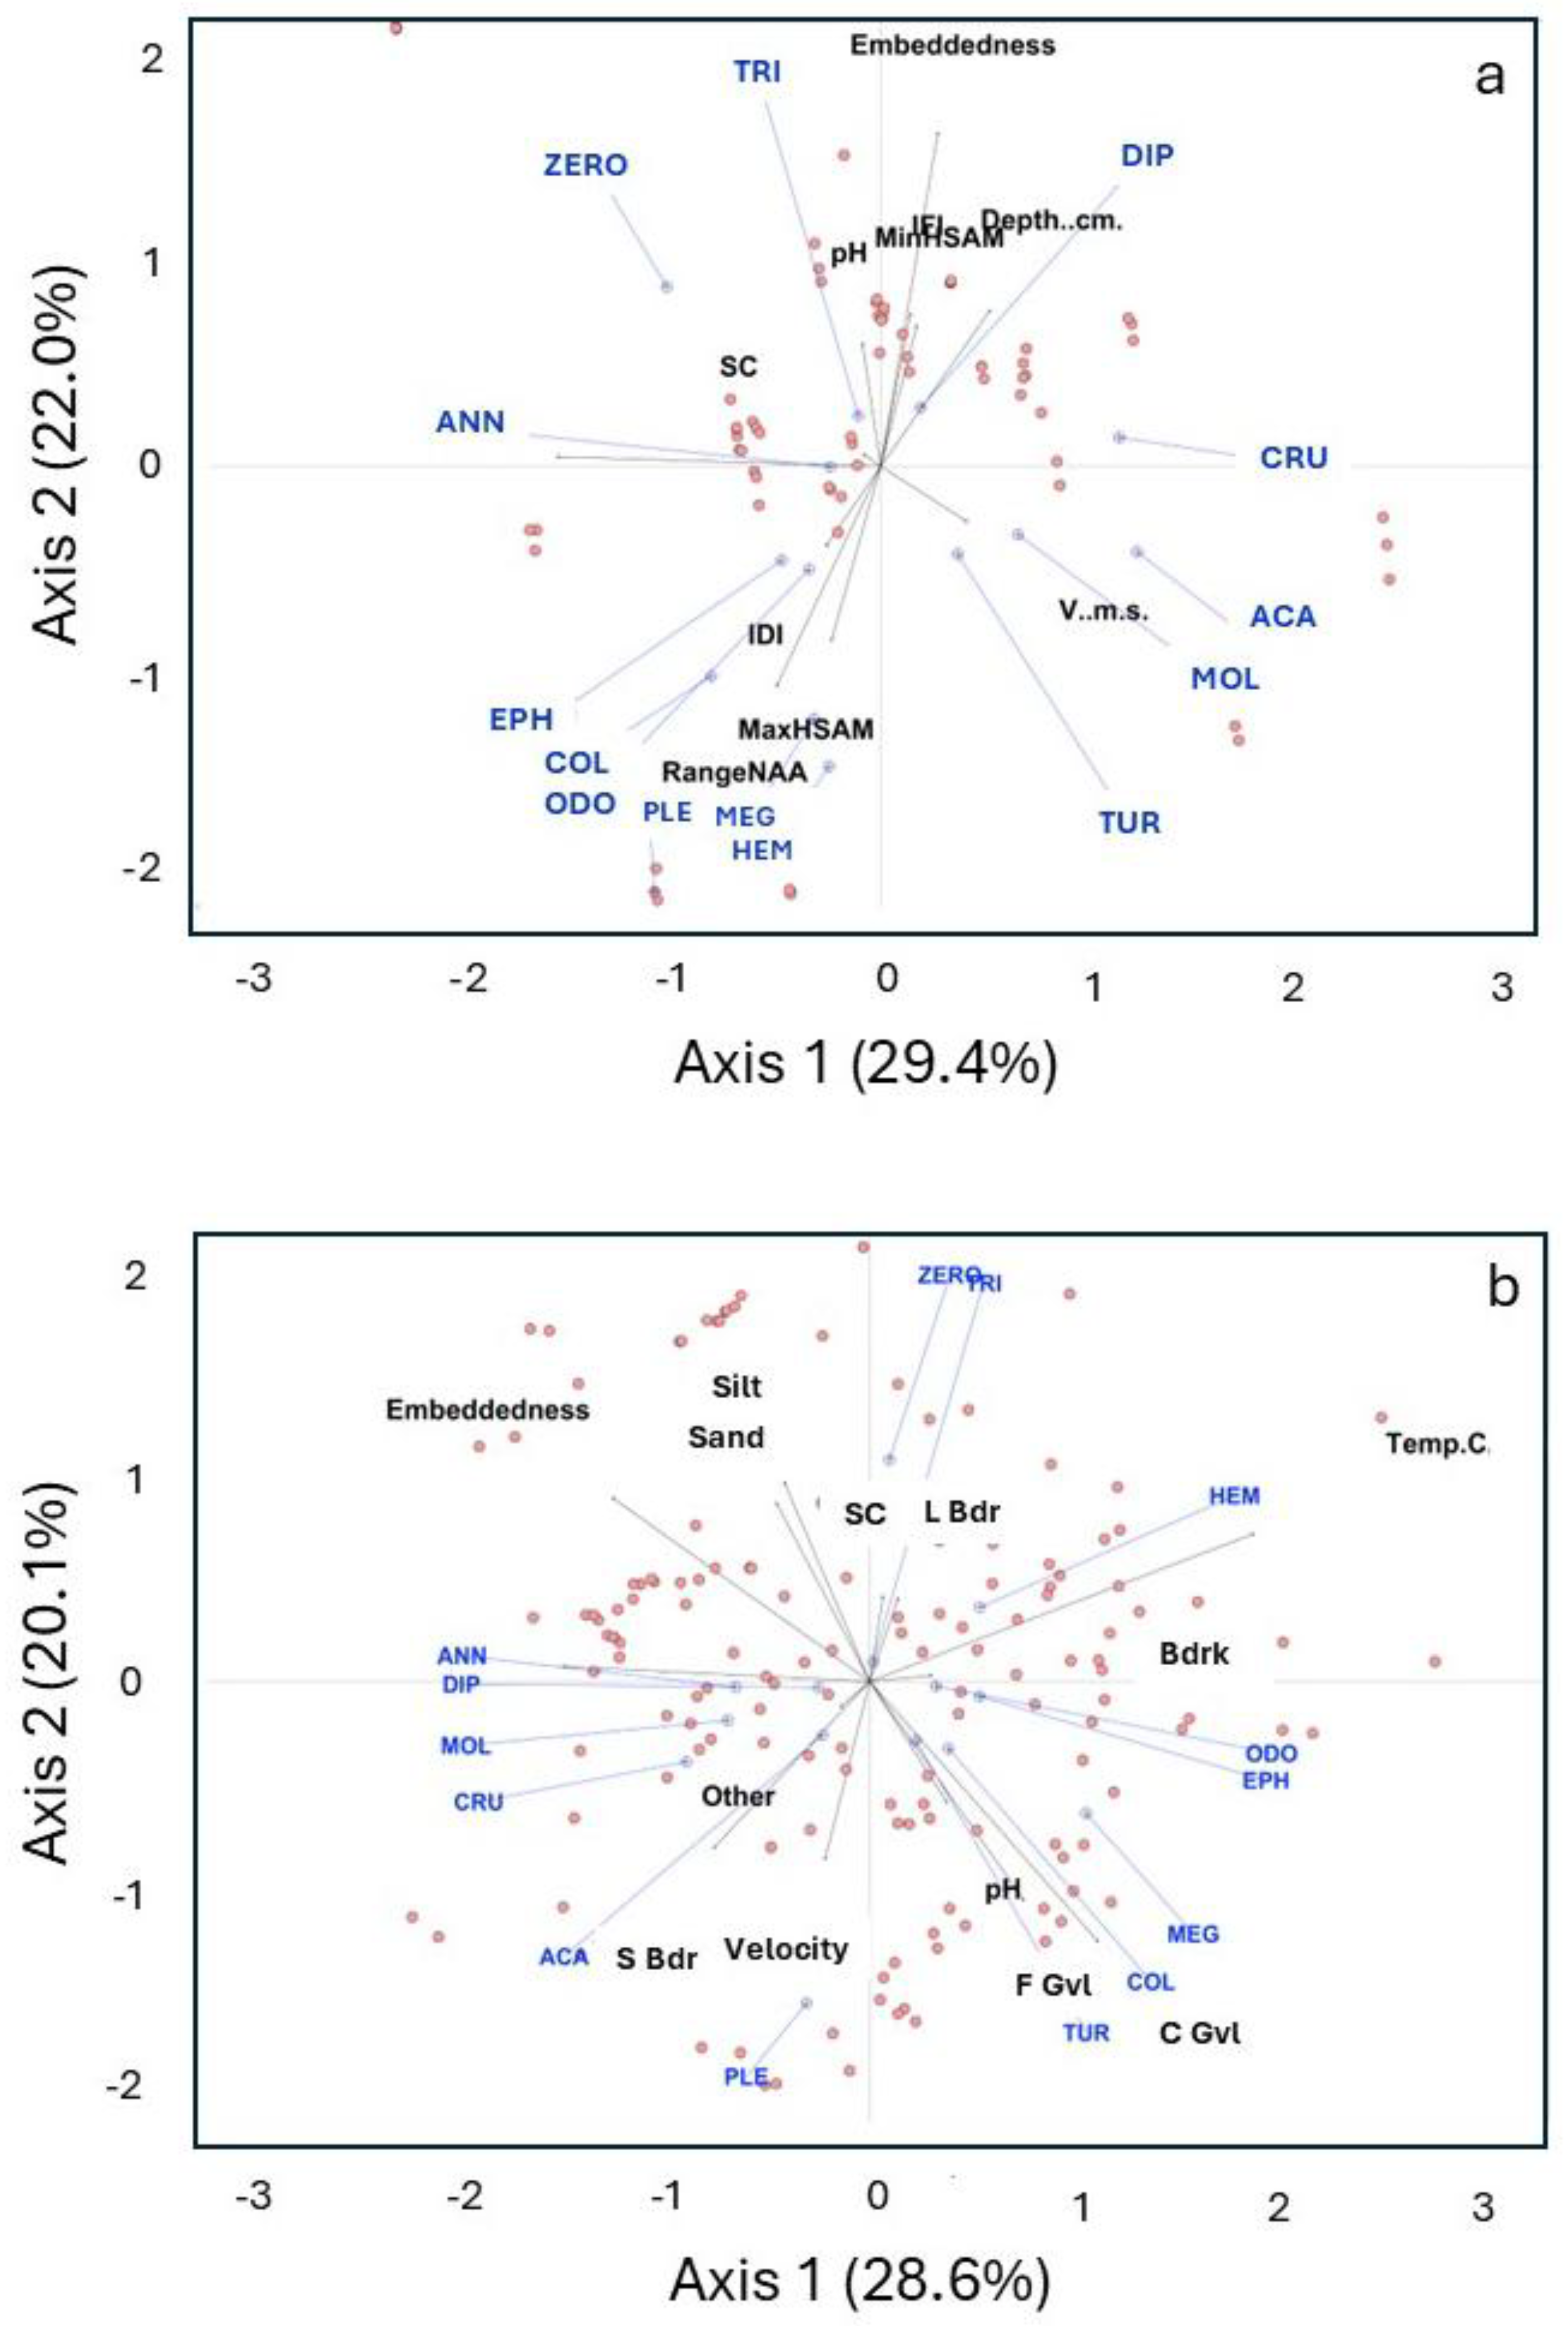
The first CCA demonstrated the degree to which AMI taxa were associated with variation in hydrologic regime and its influences on embeddedness, as well as geochemistry (Figure 6a). The abscissa (RD Axis 1) explained 29.4% of this constrained variation (eigenvalue 0.157, p = 0.020), and Axis 2 explained 22.0% (eigenvalue 0.110, p = 0.219). In combination, the axes explained 51.4% of total inertia, a highly significant value indicating significant correlation between aquatic invertebrate composition and coupled hydraulic and substratum characteristics (p = 0.001; Monte Carlo permutation test, n = 999; F = 1.577). Sites characterized by high hydrologic variability (rNAA and maxHSAM) were strongly associated with unembedded substrata and increased density of Ephemeroptera, Coleoptera, Odonata, Plecoptera, and Megaloptera. In contrast, sites characterized by hydrologic stability (low rNAA, and maxHSAM) and geochemical enrichment had high levels of calcium carbonate cementation that encrusted and sealed benthic substrata (e.g., the Paria and Little Colorado Rivers, Nankoweap and Havasu Creeks) were dominated by Diptera or supported no AMI (e.g., Chuar Creek, Pumpkin Spring). Analogously, tributaries and confluences that were embedded in silt and sand commonly supported few AMI, primarily case-dragging Trichoptera, surface-dwelling Hemiptera, Mollusca, Annelida, and Chironomus, and other nematoceran Diptera (Figure 4 and Figure 6). The water-temperature gradient was aligned perpendicular to the fine-coarse sediment gradient axis.
The second CCA demonstrated the degree to which benthic macro-invertebrate taxa were associated with different benthic substratum grain sizes (Figure 6b). The abscissa (RD Axis 1) explained 28.6% of this constrained variation (eigenvalue = 0.343, p = 0.016), while Axis 2 explained 20.1% (eigenvalue = 0.257, p = 0.083), together explaining 48.7% of the total inertia, another highly significant value that indicated a significant correlation between aquatic invertebrate composition and substrate characteristics (p = 0.001; Monte Carlo permutation test, n = 999; F = 1.956). In this ordination, embeddedness is aligned with fine substrata (i.e., silt and sand) and contrary to the axis of loose gravels (fine and coarse gravel classes), as well as pH. High levels of embeddedness were occupied by ooze-dwelling worms, Chironomus midge larvae, microcrustaceans, or had no AMI (Zero), while low levels of embeddedness were associated with Odonata (particularly Coenagrionidae), as well as Hemiptera, Ephemeroptera, Megaloptera, Coleoptera, and planariid flatworms (Appendix A). As in the first CCA, the water-temperature gradient was aligned perpendicular to the fine-coarse sediment gradient axis.
The mean Dmag scores among 24 Grand Canyon tributaries was 0.31 (95% confidence interval = 0.262; Table 1); however, Dmag scores ranged widely from −1.0 to 0.88. As cementation increased from low to high levels, mean Dmag decreased from 0.43 to −0.60. Similarly, as embeddedness changed from low to high levels, Dmag decreased from 0.51 to −0.03. Both trends were highly variable due to tributary-specific differences in dissolved and suspended sediment loads. As demonstrated through the CCA analyses, tributaries with low cementation and a diverse mix of gravels and cobbles supported larger and more species-rich AMI assemblages and higher Dmag scores (e.g., Bright Angel Creek, Dmag = 0.88, and Royal Arch, Stone, Deer, and Tapeats Creeks all had Dmag values > 0.65). In contrast, tributaries with extensive channel-floor cementation supported low and sometimes negative Dmag scores. In all, seven (33.3%) of the tributaries had negative Dmag scores, with low to minimal AMI species richness (e.g., Paria and Little Colorado Rivers, Pumpkin Spring; Table 1). However, the overall positive Dmag score among all Grand Canyon tributaries indicated the generally more robust AMI faunal assemblage in tributaries than in the mainstream.
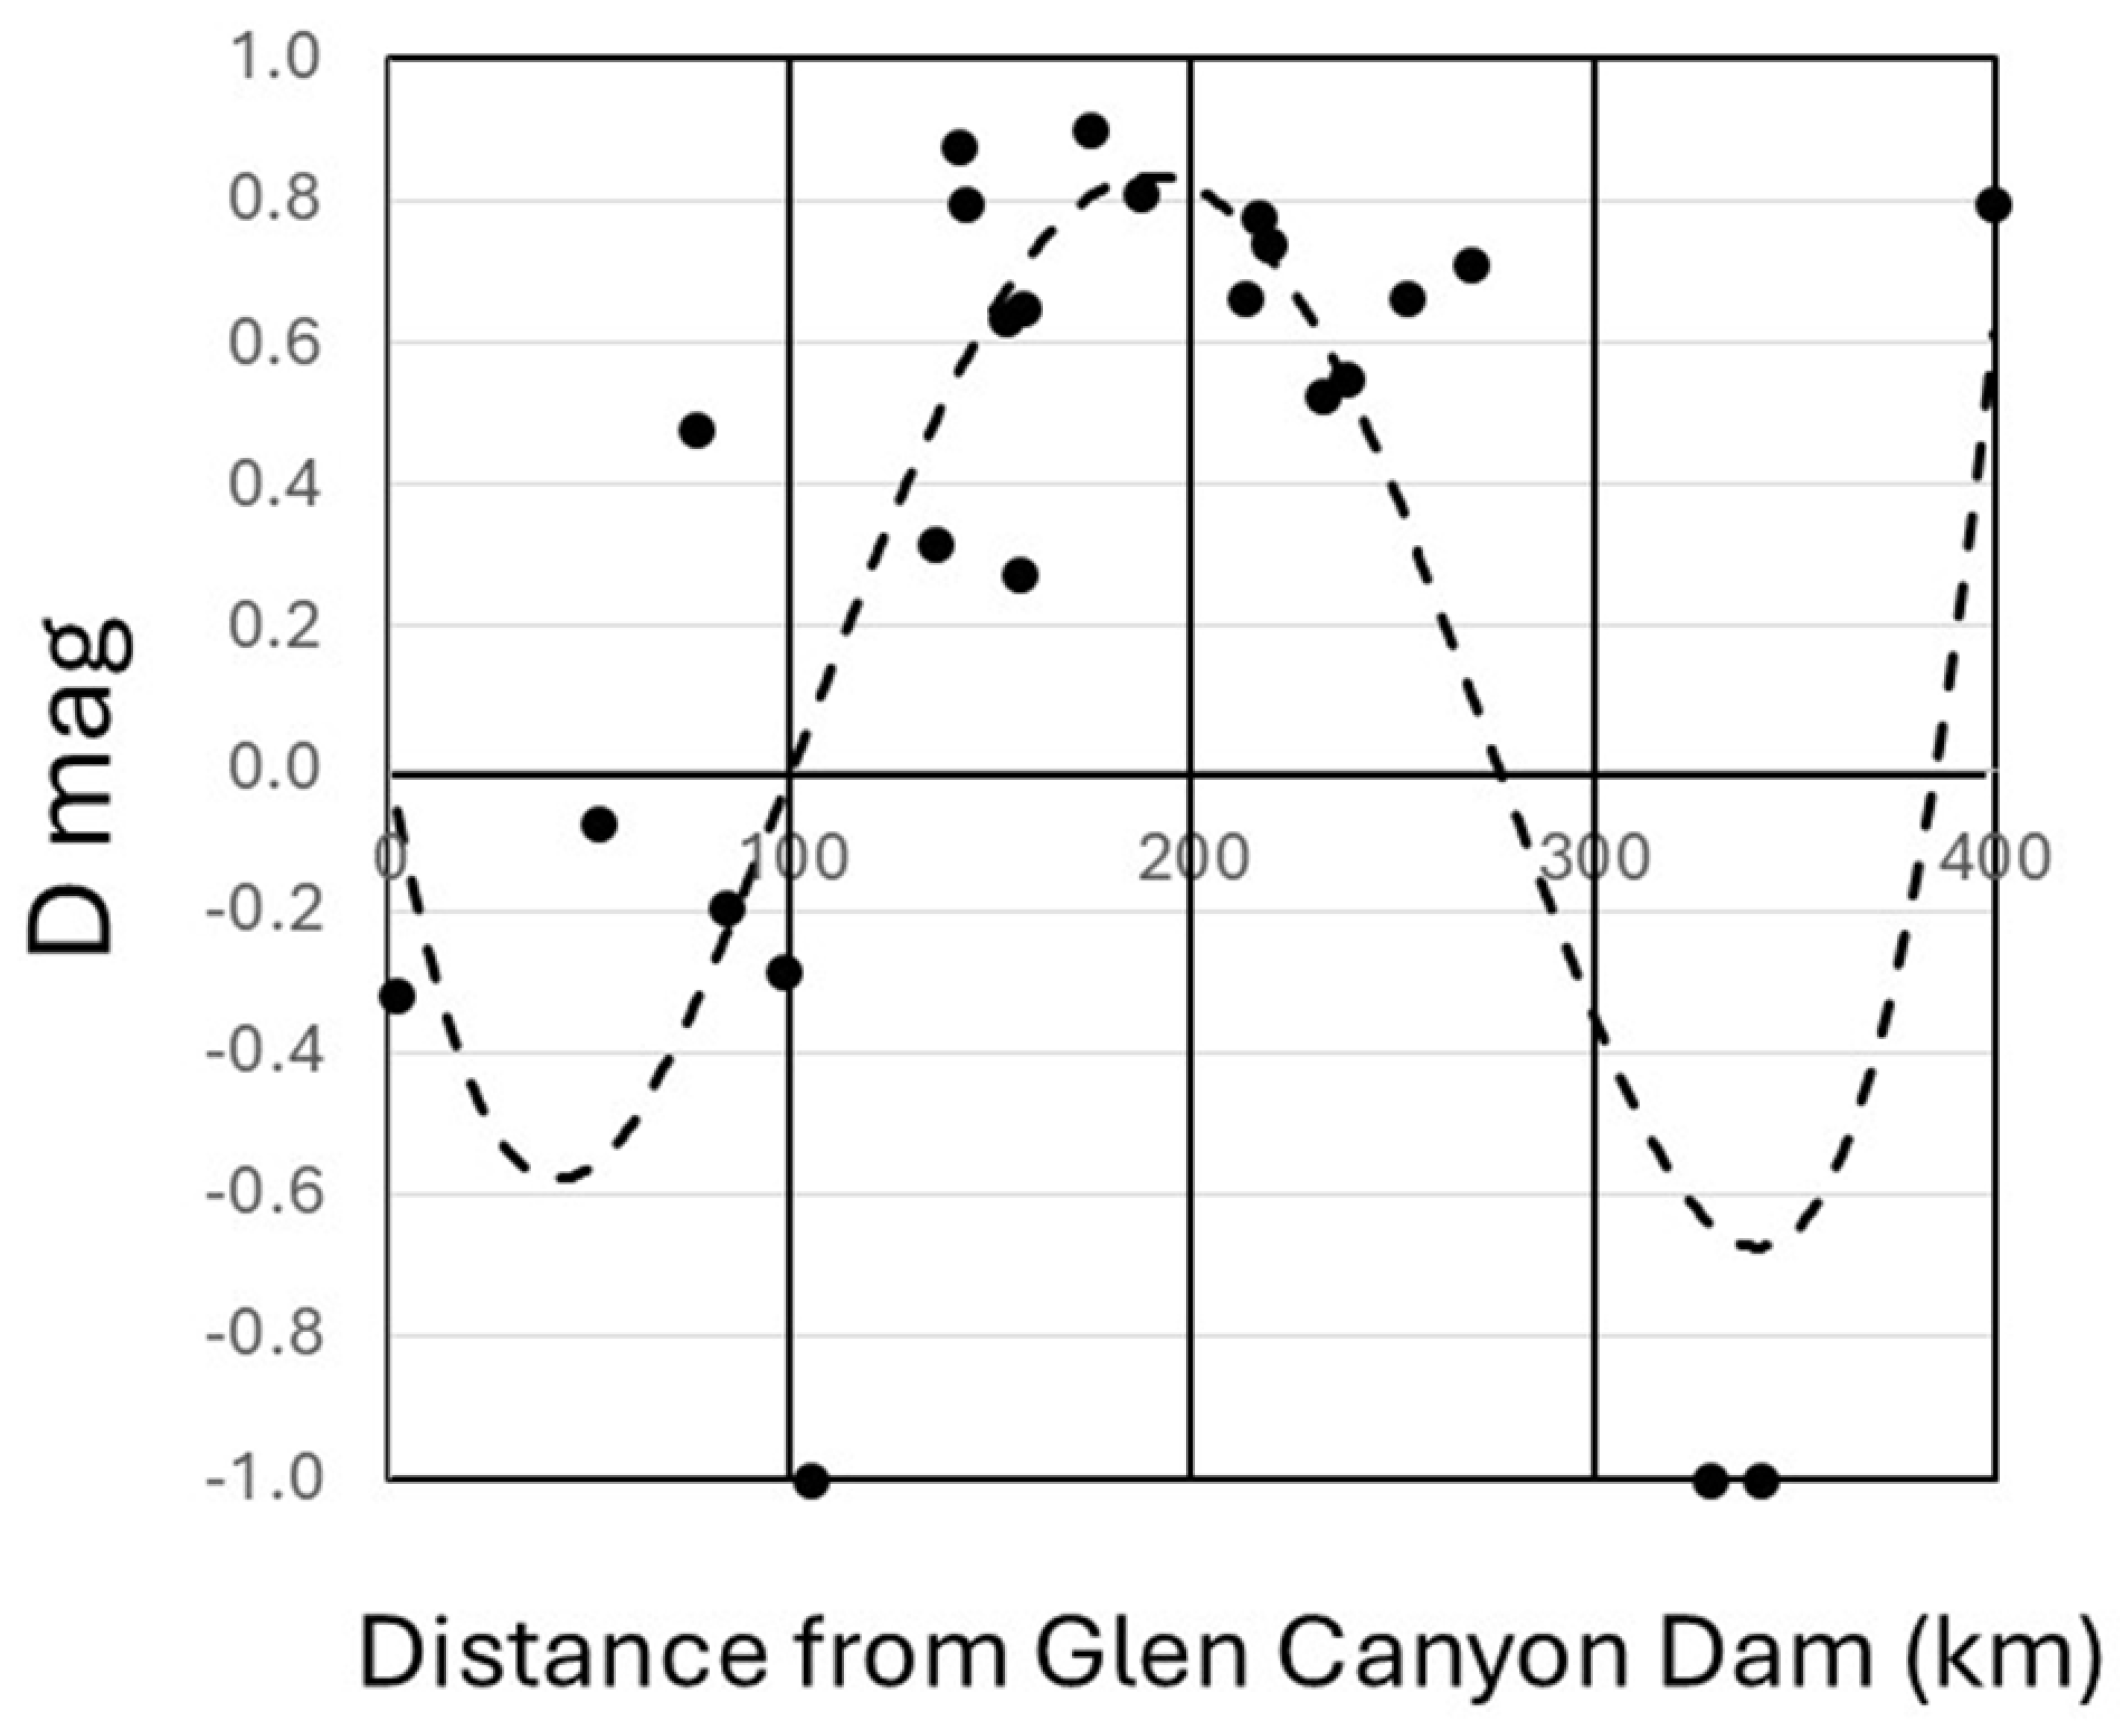
Dmag was non-linearly related to distance from Glen Canyon Dam (4th-order polynomial R2 = 0.631) but in the reverse pattern of electrical conductance, with maximum values in the middle reaches and lowest values at distances near the dam and downstream from the mid-Canyon Muav Gorge (Figure 7; [1]), except for the karstic discharge of lower- Canyon Surprise Canyon Creek. Dmag did not vary by basin area (best fit, 3rd-order polynomial R2 = 0.074) and neither by stream order, nor in relation to tributary water temperature or pH (R2 values < 0.11 and <0.02, respectively).
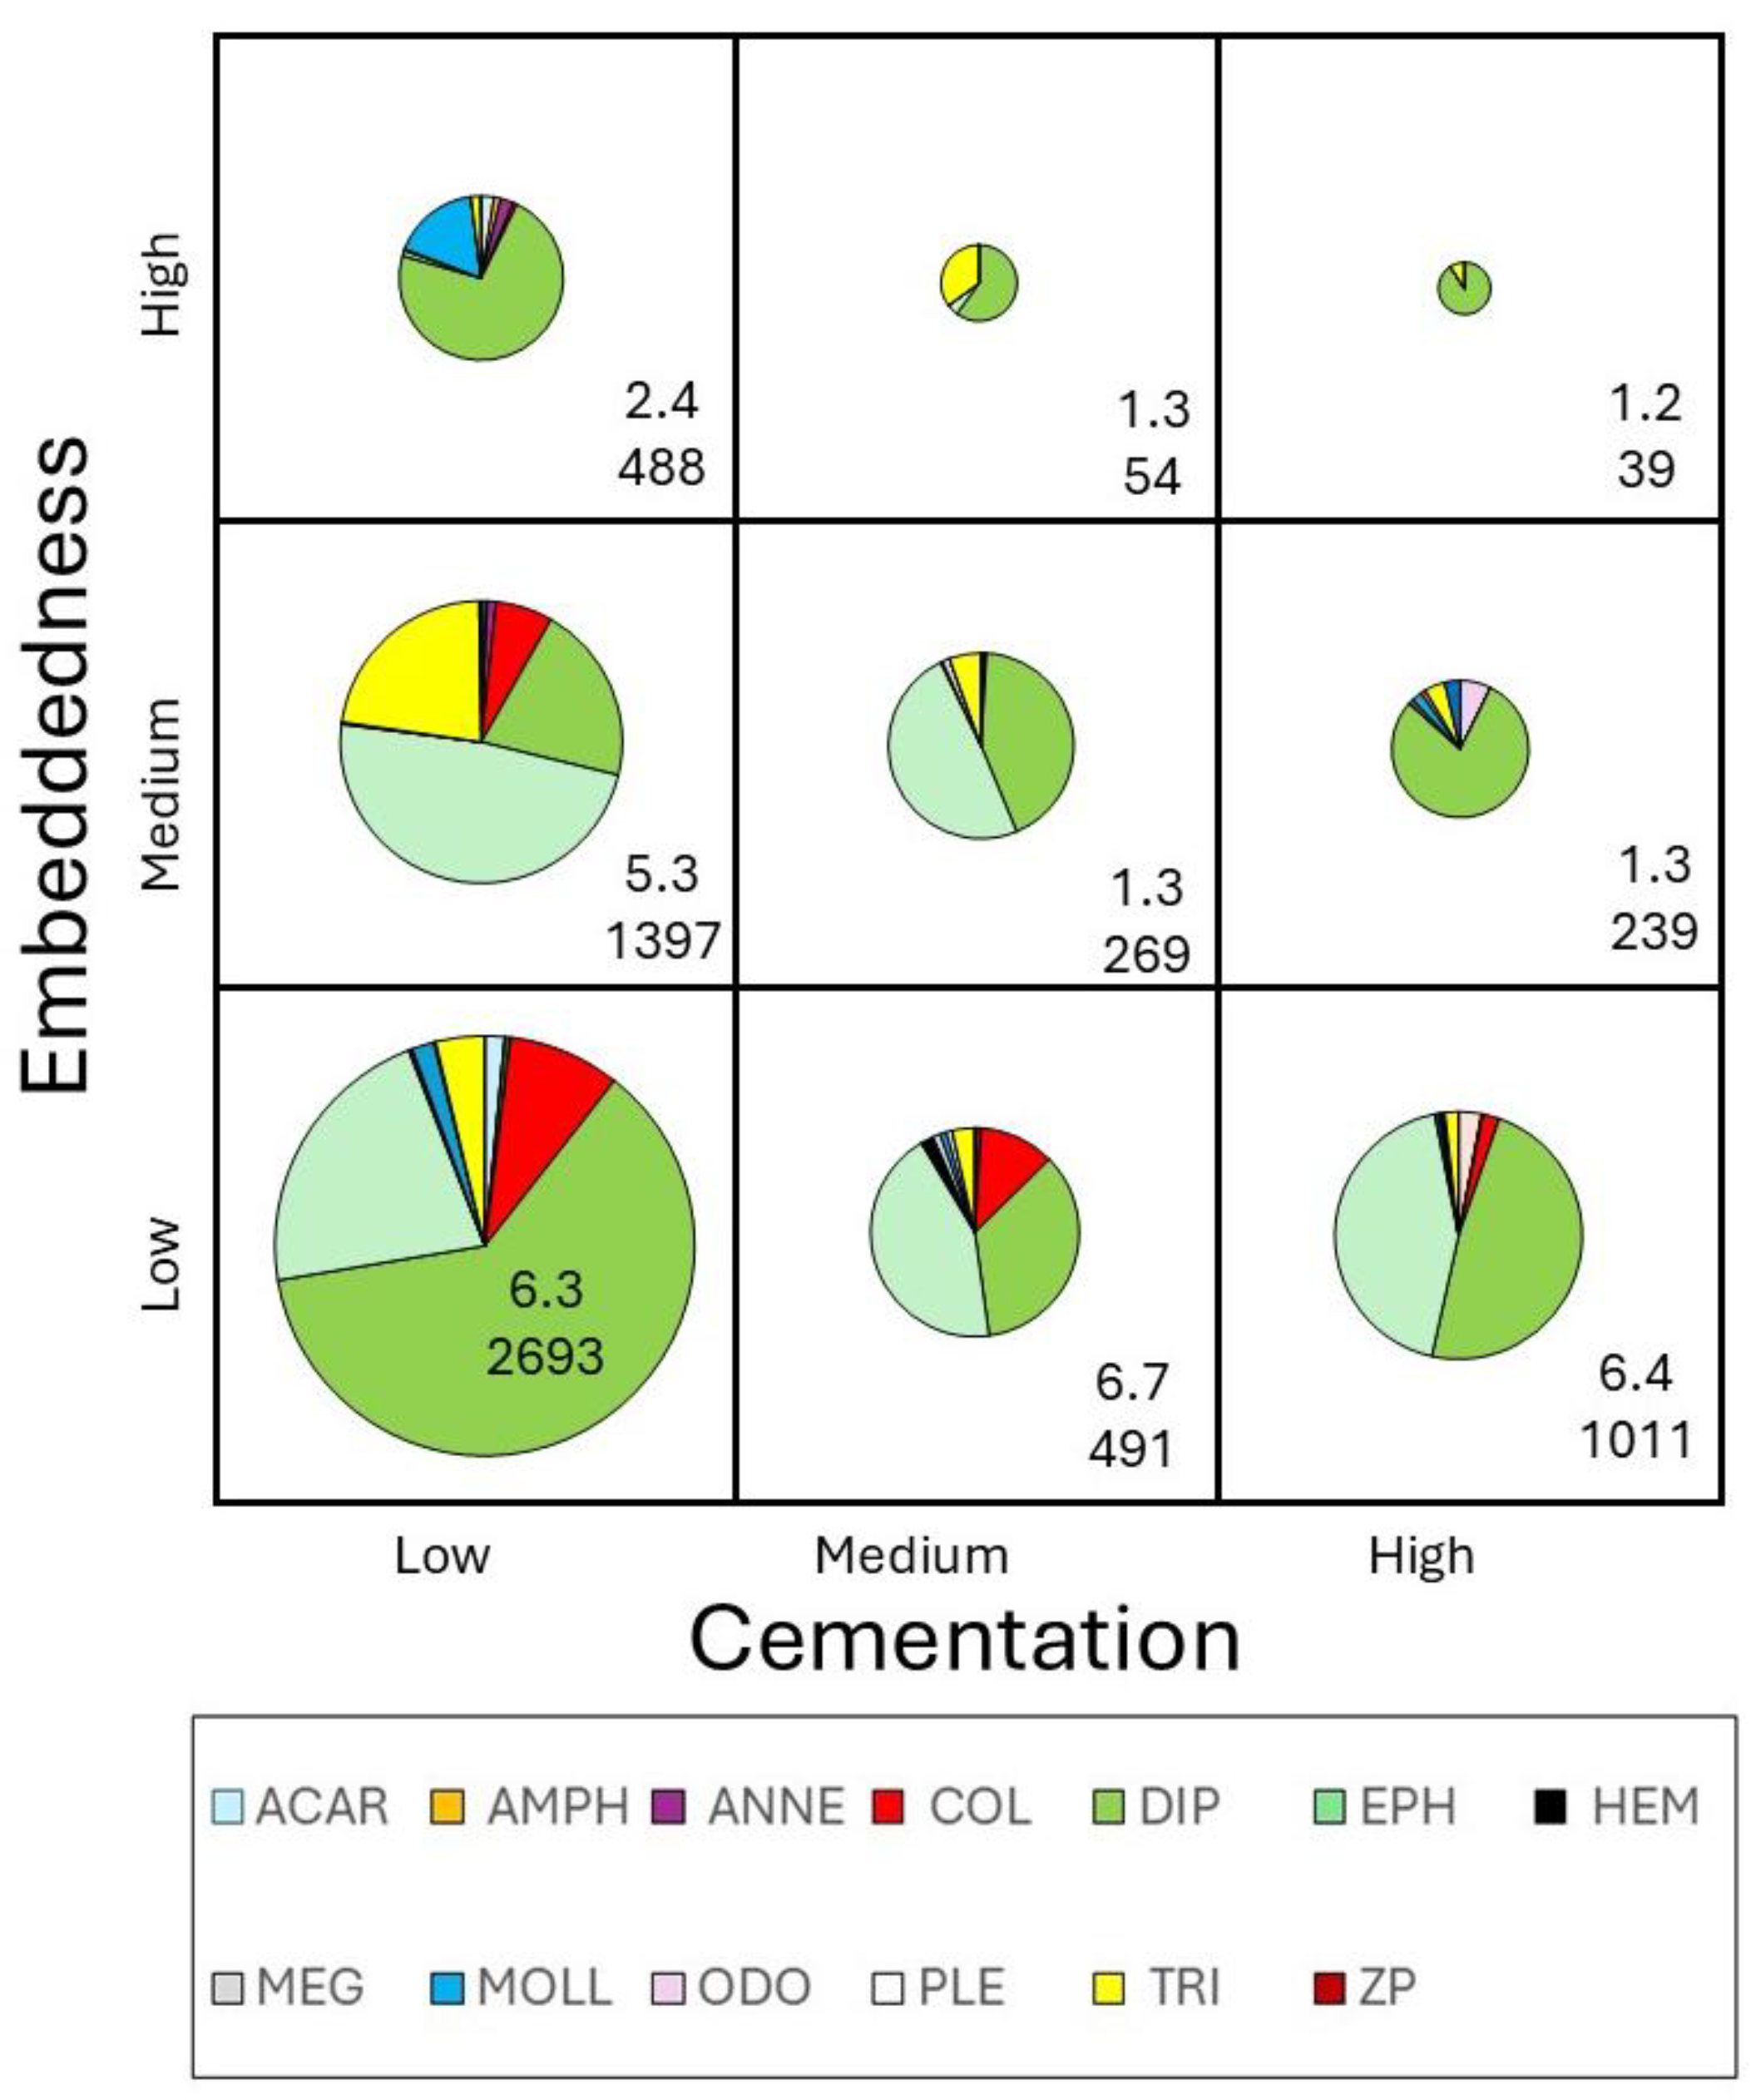
AMI density/m2 across cementation and embeddedness gradients supported the hypothesis that aquatic macroinvertebrate assemblages are negatively related to elevated values and intensified interaction effects between cementation and embeddedness (Figure 8). Density decreased 2.7-fold from low-to-high cementation estimates, 6.1-fold from low-to-high embeddedness estimates, and decreased 136.0-fold across the diagonal low-to-high gradient interaction axis. The mainstream AMI fauna was, as expected, depauperate and primarily limited to Chironomidae, Gammarus lacustris, Physidae, and Potamopyrgus antipodarum. Our data indicated that AMI assemblages were less responsive to cementation than to embeddedness. Chironomidae (Diptera) and Baetid (Ephemeroptera) dominated the tributary fauna, with the latter somewhat increasing in dominance at intermediate to higher levels of both gradients in tributaries, but not occurring in the mainstream. In contrast, tributary elmid beetles and larval Plecoptera occurred at the lowest levels of both gradients, while larval Corydalus texanus Megaloptera and both larval and adult aquatic dytiscid and hydrophilid Coleoptera occurred at low-to-medium levels of those tributary gradients.
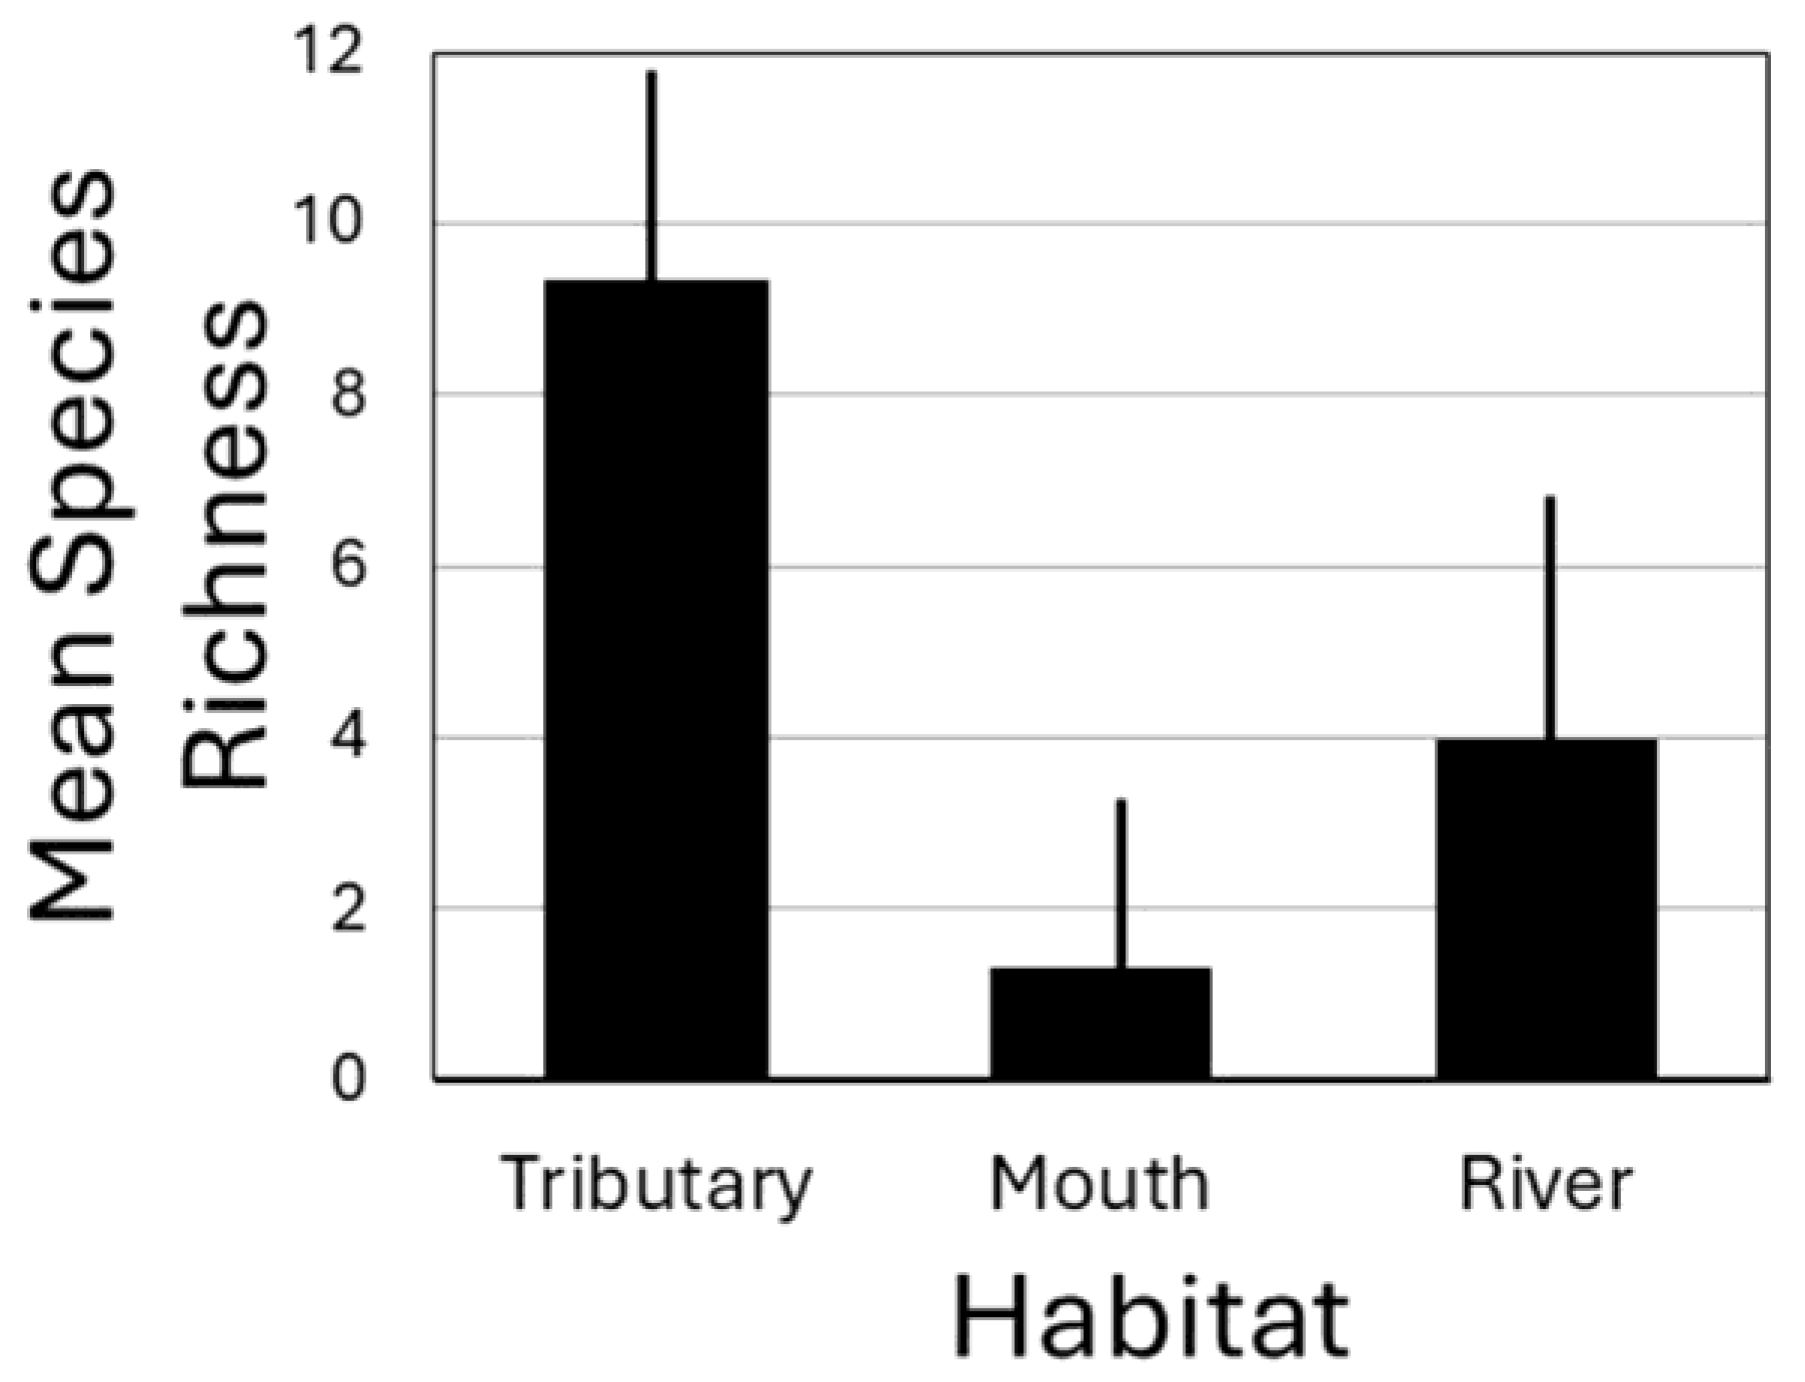
Woodbury’s [29] pre-dam data on the aquatic insect (AQI) fauna of the 290 km-long Glen Canyon basin immediately upstream from Grand Canyon revealed a grand mean of 9.33 species/site among thirty-three tributary sites versus 4.00 species/site among seven mainstream sites (Figure 9). Glen Canyon tributaries supported a total of 86 (92.5%) of the 93 AQI taxa detected, of which 73 (79.3%) were found only in tributaries, 11 (12%) were detected only in the river, 8 (8.7%) co-occurred in both tributaries and the mainstream, and 2 taxa were unique to tributary mouths (Hydrophilus triangularis and Culex mosquitoes). All except 1 of 15 taxa (an ooze-dwelling Polypedilum chironomid) occurring in confluence zones were also found in tributaries, while only one species (a Callibaetis mayfly) co-occurred in both confluences and mainstream habitats. Woodbury repeatedly described the mainstream as virtually devoid of insect life except at the few cobble, gravel, or wood deposits near tributary mouths. The tributaries his crew sampled were rich in AMIs, except in streams and confluence zones that were highly embedded in fine sand or ooze (e.g., the San Juan and Dirty Devil Rivers). These data generated a Glen Canyon basin-wide Dmag score of 0.82, indicating vastly greater AQI species richness in the tributaries than in the pre-dam mainstream, as described by Woodbury.

4. Discussion

Our predictions and conceptual model on the hierarchical impacts of hydrography and geochemistry on benthic AMI assemblage complexity were largely supported. AMI TMDs are now common in the post-dam Colorado River downstream from Glen Canyon Dam, and our review of Woodbury’s [29] data indicates that TMDs were prevalent in the pre-dam Glen Canyon Basin upstream as well. TMDs arise from differences between mainstream versus tributary hydrology and geochemistry, interactions that dictate levels of benthic embeddedness and channel-floor cementation, respectively. The resulting substrate conditions influence AMI and their habitat and refuge distribution, assemblage composition, and density (Table 2; Figure 6), with cementation, fine sand deposition, and their interactions reducing AMI assemblage complexity (Figure 8). Dmag values reflect the magnitude and directionality of AMI TMDs, with elevated levels of either or both processes limiting AMI assemblage complexity. We and Woodbury report several examples of near-natural Colorado River tributaries with virtual sterility to complex, species-rich assemblages in comparison with the adjacent mainstream. These patterns extend the application of Ward and Stanford’s [3] serial discontinuity concept to include natural and well as regulated streams and confluence zones. Our findings support context dependency among factors that contribute to AMI assemblage complexity [6] and the hierarchical causality of TMD development arising from physical factor interactions, as reviewed by Dye [9].
At coarse spatio-temporal scales, interactions among catchment-based, hydrography-related embedding of firm substrata in mainstream-deposited fine sand and aquifer-based geochemical carbonate cementation of tributary channel floors control AMI microhabitat suitability and refuge availability (Figure 1, Figure 4 and Figure 8). We found few AMIs where channel floors were embedded in fine sediments (e.g., in the mainstream in general and in the confluence zones of Kanab Creek and the Paria River). Mainstream floods in sand-dominated rivers scour and redeposit fine sediments, burying benthic substrata in sand and eliminating benthic refugia. Nearly all mainstream sites in Grand Canyon and in the pre-dam mainstream in Glen Canyon were floored by sand or had cobbles and boulders embedded in fine sand, with no discernible or reported cementation (Table S1) [29].
Like embeddedness, precipitate cementation reduced the availability of AMI benthic refugia (Table 2; Figure 6). Conductance and water temperature varied widely among Grand Canyon tributaries, ranging from low values in karstic springbrooks (e.g., Bright Angel, Tapeats, and Deer Creeks), to medium levels (e.g., Kanab Creek), to high levels in springbrooks emerging from Precambrian bedrock or in shale-dominated basins (e.g., Nankoweap, Chuar, and Havasu Creeks, and the Paria and Little Colorado Rivers). AMI assemblages were sparse and depauperate at high levels of benthic carbonate cementation: we found few to no AMI in streams with elevated to extreme conductance that were heavily cemented by calcium deposition (e.g., the travertine-depositing Havasu Creek, the Little Colorado River, Pumpkin Spring; Figure 8). In such settings, the AMI assemblages were dominated by Diptera (primarily Chironomidae, particularly Chironomus blood worms), tipulid crane fly larvae, and Mollusca (primarily nonnative Potomopyrgus antipodarum, along with physid snails of unknown nativity). Rundio [42] similarly reported lower AMI species richness in travertine-depositing streams in California, and Sada and Thomas [43] concluded that electrical conductivity exerted the strongest impacts on aquatic invertebrate assemblages in springbrooks across elevation in the Great Basin and Mojave Deserts in southwestern USA. In great contrast to precipitate-depositing streams, unembedded, low-conductance karstic streams in Grand Canyon supported complex AMI assemblages of Plecoptera, aquatic Hemiptera, Corydalus texanus Megaloptera, Coleoptera such as Microcylloepus elmids, and other taxa that require hyporheic interstitial space.
Several implications of our hydrographic analyses warrant further elucidation. Flood peak timing varies between tributaries and the mainstream in the central Colorado River basin. Tributary spates regularly occur in relation to late winter–early spring snowmelt on the surrounding plateaus, and again in relation to mid–late summer monsoonal rains, with rare, erratic winter rain-on-snow events; see, e.g., [24]. This flood phenology provides a sediment and nutrient pulse to tributaries early in the growing season, likely enriching primary producer and primary and secondary consumer production during the May–June dry season when solar radiation reaches its zenith [17,21,44]. While spates scour and reset substrate composition, the availability of benthic AMI refugia may be short-lived if stream geochemistry results in rapid re-cementation. Oberlin et al. [13] attributed variation among tributary AMI assemblages primarily to catchment area (stream order), a conclusion for which we found little support (linear regression of AMI richness to basin area R2 = 0.074). Rather, we report that benthic habitat suitability was the primary determinant of AMI assemblage complexity in the streams we studied.
In considerable contrast to tributaries, pre-dam mainstream floods typically occurred as a result of snowmelt in the distant Rocky Mountains, arriving with great variability in early to mid-summer (June to early August) [21]. Pre-dam mainstream floods impounded tributary mouths, creating (depending on geomorphology and slope angle) potentially large pools of clear, warm water at tributary mouths during early summer, corresponding to the primary period for larval fish development. L.E.S. (unpublished data) observed this phenomenon during the post-dam peak flows of 1983–1986 at the mouths of many Grand Canyon tributaries. For example, the flood-impounded mouth of the Little Colorado River extended more than a kilometer upstream into that drainage, an observation corroborated by Protiva et al. [45]. As mainstream floods subsided, fine sand was deposited in confluence zones, in some cases damming tributary mouths and embedding firm benthic substrata there in silt and sand. The difference in pre-dam peak flow arrival between tributaries and the mainstream led to impoundment of tributary mouths. This formerly common phenomenon that likely strongly affected slack-water habitat area and clarity, thermal and nutrient dynamics, AMI distribution, and fish reproduction in confluence zone hotspots of fluvial ecosystem productivity [11].
Tributary confluence habitats revealed TMD causal mechanisms. AMI species richness and density in Grand Canyon tributaries generally progressively decreased from the tributary into the mainstream, as Hofknecht [12] reported. However, stepwise reduction was not always evident: the confluence zones of larger, low-gradient tributaries supported limited AMI density and complexity (e.g., the mouths of the Paria and Little Colorado Rivers and Kanab Creek) due to the deposition of silt and organic ooze that precluded occupation by most AMIs.
Episodic flood scour that reduces tributary floor cementation temporarily provides interstitial refugial space for AMI. But over the subsequent weeks to months that cementation redevelops, eliminating benthic refugial habitat, probably resulting in an as-yet-unstudied AMI assemblage transition. In contrast to their parent streams, confluence zone habitats are subject to both spate-related and erratic tributary flooding as well as regular to occasional inundation by mainstream flows. These interactions dilute, retard, or prevent cementation, and high mainstream flows deposit fine sand, sometimes damming low-gradient tributary mouths.
Our results at the Tapeats Creek confluence [2] and Woodbury’s 1959 data [29] revealed that the mouths of low-gradient tributaries were commonly dominated by fine sediment and organic ooze deposits. Such deposition, particularly occurring during springtime mainstream spates and in Glen Canyon, typically resulted in lower AMI richness and density in confluence zones compared to either of those in the tributary or the adjacent mainstream. Woodbury [29] noted that thick ooze deposits at the mouths of several pre-impoundment Glen Canyon tributaries supported no aquatic insects (e.g., the mouth of the Escalante River), and we report similar conditions in post-dam Grand Canyon at the mouths of the Paria and Little Colorado Rivers and Chuar and Kanab Creeks in Grand Canyon. Those tributaries all drain shale-dominated basins and their low-gradient silt-choked confluence zones support low AMI species richness and density. In contrast, the mouths of most cool-water, low-conductance tributary streams supported greater AMI density and richness than did their parent streams, particularly those tributaries with steep channel slopes and strong lotic flow. Greater AMI assemblage complexity at the mouths of Tapeats and Bright Angel Creeks in comparison with those of their parent tributaries may additionally reflect intermediate disturbance dynamics [2,32,33,34].
Our analysis of pre-dam aquatic insect distribution in perennial streams in the Glen Canyon basin [29] revealed that TMDs occurred naturally in that portion of the Colorado River basin. The basin-wide Dmag score of 0.82 there indicated that tributary AQI assemblages were greatly enriched in comparison to those in the mainstream Colorado River. Only seven species were unique to the mainstream, and only one species was found in common in tributary mouths and the mainstream. In contrast, the average Dmag score across all post-dam Grand Canyon tributaries was 0.31, reflecting the great diversity of tributary geochemistry and fine sediment transport.
By virtue of the sand-dominated mainstream sediment conditions that characterized Glen and Grand Canyon prior to impoundment and still prevail in Grand Canyon [14,21,25], Woodbury’s 1959 data [29] suggest that TMDs were likely to have been prevalent in the pre-dam Colorado River corridor in Grand Canyon. While Woodbury reported little overlap of tributary and mainstream aquatic insect assemblages, and even lower overlap in tributary confluence habitats, we report that 30.4% of the AMI taxa detected in post-dam Grand Canyon tributaries were found in tributary mouths. This suggests that flow regulation, and perhaps particularly post-dam reduced mainstream turbidity, may have enhanced AMI species richness and density among Grand Canyon tributary mouths, and therefore improved fisheries’ foodbase production in confluence zones. Such a finding supports Thorp and Delong’s river productivity model [11], in which patchily distributed fluvial hotspots substantially contribute to overall river productivity. This also supports Green et al.’s [6] proposition that context dependence among physical and niche selection controls riverine AMI biodiversity.
Although not studied here, we observed that inner-canyon and particularly North Rim wildfires reduce tributary AMI and fisheries’ habitat quality, sometimes to the point of eliminating those assemblages altogether. Given the remoteness of Grand Canyon tributaries and the lack of connectivity to the mainstream described here, wildfire impacts from post-fire ash flow embeddedness and anoxia can devastate AMI assemblages (see, e.g., [46]). Such impacts are likely to precipitate species loss and AMI successional development, a process that may decelerate or become increasingly imbalanced through repeated or more severe fires, in accordance with ecological disturbance and climate change theory [32,33,34].

5. Conclusions

We report that TMDs are common in the regulated Colorado River, with AMI assemblage complexity negatively related to carbonate cementation and to fine sand embeddedness gradients, both individually and in concert. Our conceptual model (Figure 2) was supported by AMI distribution data (Figure 8), and evidence of TMDs was also found in Woodbury’s 1959 aquatic insect data from the pre-dam Glen Canyon section of the Colorado River upstream from Grand Canyon [29]. The common occurrence of TMDs in Grand Canyon was documented empirically, through multivariate analyses, and through analysis of Dmag analysis. Rather than single-factor controls on AMI (e.g., fluctuating flows, mainstream water temperature, tributary basin size or extent, or geochemistry), as has been previously proposed, we posit that Colorado River AMI assemblages are more strongly regulated by benthic substrate complexity and refugial habitat availability in relation to the life histories of associated AMI.
The regulated Grand Canyon section of the Colorado River is presently managed both for fine sediment to maintain riverside camping beaches and for protected native species and desired nonnative rainbow trout (Oncorhynchus mykiss) [25]. Our findings lend further support to previous research [2] that no single flow regime in Grand Canyon can maximize both fine sediment mass balance and AMI primary and secondary production. Our results expand the context of the serial discontinuity model [3] to include tributary discontinuities in natural as well as regulated rivers, and indicate that some, but not all tributary confluences function as hotspots of instream production [11], supporting the mixed-factor causality of TMD development reviewed by Dye [9]. Thus, our study provides basic insight into fluvial ecosystem ecology, as well as insight into a more nuanced ecological understanding of aquatic foodbase management options in both natural and regulated rivers.

Supplementary Materials

The following supporting information can be downloaded at: https://www.mdpi.com/article/10.3390/w18030395/s1, Table S1: master dataset; Table S2: Dmag tests. R code is available on reasonable request.

Author Contributions

Conceptualization, L.E.S. and C.E.; Methodology, L.E.S. and J.H.H.; Software, J.H.H.; Validation, L.E.S. and J.H.H.; Formal Analysis, L.E.S. and J.H.H.; Investigation, L.E.S. and C.E.; Resources, L.E.S.; Data Curation, L.E.S. and J.H.H.; Writing—Original Draft Preparation, L.E.S.; Writing—Review and Editing, All; Visualization, Supervision, Project Administration, and Funding Acquisition, L.E.S. All authors have read and agreed to the published version of the manuscript.

Funding

Partial funding for this project was provided by Argonne National Laboratories to Springs Stewardship Institute under Contract No. 3F-60173, with additional support from the Grand Canyon River Outfitters Association.

Data Availability Statement

Data from this project are provided in the Supplementary Materials (above) and are available from the corresponding author upon request.

Acknowledgments

This project was conducted under National Park Service scientific research and collecting permits GRCA-2023-SCI-0020, GRCA-2024-SCI-0032, and GRCA-2025-0009. We thank Argonne National Laboratories for funding and administrative oversight through ANL Contract No. 3F-60173 to the Springs Stewardship Institute, and we thank Western Area Power Administration for project support and oversight. We kindly thank Grand Canyon River Outfitters Association for support for Springs Stewardship Institute research through the Grand Canyon Fund, and Grand Canyon Youth and its enthusiastic student participants, as well as the US Geological Survey Grand Canyon Monitoring and Research Center and its staff for field assistance and logistics. K. Cooney provided USGS data on Little Colorado River water quality. Jeri Ledbetter and Izzie Speer provided much-appreciated administrative support at Springs Stewardship Institute. James Franklin and Nadia Damra provided SSI sample sorting and enumeration assistance, and Jeff Jenness provided map production. This project required no special security other than compliance with US Coast Guard and National Park Service boating regulations and compliance with USGS and Grand Canyon Youth guidelines. No artificial intelligence was used in the preparation of this report.

Conflicts of Interest

The authors declare that this study was funded by the US Department of Energy through Argonne National Laboratories, with additional funding from the Grand Canyon River Outfitters Association, Inc. The funders were not involved in the study design, collection, analysis, interpretation of data, the writing of this article or the decision to submit it for publication.

Appendix A

Aquatic invertebrates detected: project total (11,365), relative frequency in tributaries, in confluence zones, and in the mainstream Colorado River in Grand Canyon.
Abbrev.Higher TaxonMorpho-TaxonTotal IndividsTributary Rel FreqConfluence Zone Rel FreqRiver Rel FreqTotal Freq
ACAAcarinaHydrachnidia 2 spp.1911.5740.4920.7010.017
AMPAmphipodaGammaridae290.0140.0340.3880.003
ANNAnnelidaAnnelida 3 spp.910.4250.2200.7010.008
COLColeopteraChrysomelidae10.0000.0000.0000.000
COLColeopteraDytiscidae130.1780.0000.0000.001
COLColeopteraElmidae5796.7261.3320.1490.051
COLColeopteraHydrophilidae 5 spp.210.2470.0000.0450.002
COLColeopteraUnID Coleoptera921.0550.0370.0150.008
DIPDipteraEmpididae500.1510.5930.0600.004
DIPDipteraCeratopogonidae360.4250.0680.0150.003
DIPDipteraChironomidae 4 spp.428511.98638.13617.3230.377
DIPDipteraChironomus400.4930.0000.0600.004
DIPDipteraCulicidae 00.0000.0000.0000.000
DIPDipteraEphydridae 3 spp.260.0690.3560.0000.002
DIPDipteraPsychodidae180.2330.0000.0150.002
DIPDipteraSimuliium149018.0820.5242.0750.131
DIPDipteraStratiomyidae 2 spp. 1281.6590.1190.0000.011
DIPDipteraSyrphidae20.0270.0000.0000.000
DIPDipteraTabanidae20.0270.0000.0000.000
DIPDipteraTipuloidea 4 spp.310.2600.1690.0300.003
DIPDipteraUnID Diptera260.0680.2880.0600.002
EPHEphemeropteraBaetidae 3 spp.271726.78212.6080.2690.239
EPHEphemeropteraHeptageniidae40.0550.0000.0000.000
HEMHemipteraBelostomatidae00.0000.0000.0000.000
HEMHemipteraHEM Corixidae30.0270.0170.0000.000
HEMHemipteraHEM Veliidae300.2880.0850.0600.003
MEGMegalopteraCorydalidae310.2880.1690.0000.003
MOLHygrophiaPhysidae20.0270.0000.0000.000
MOLLittorinimorphaPotamopyrgus4161.3700.0684.6570.037
MOLMyidaDreissenidae50.0000.0170.0600.000
MOLSpheriidaSphaeriidae10.0000.0000.0150.000
ODOOdonataEnallagma40.0550.0000.0000.000
ODOOdonataLestidae30.0410.0000.0000.000
ODOOdonataLibellulidae110.1230.0340.0000.001
ODOOdonataAeshnidae60.0680.0000.0150.001
ODOOdonataCalopterygidae10.0140.0000.0000.000
ODOOdonataCoenagrionidae1240.7810.2710.7610.011
PLEPlecopteraPerlodidae40.0410.0170.0000.000
TRITrichopteraHydropsyche991.3290.0340.0000.009
TRITrichopteraHelicopsychidae10.0140.0000.0000.000
TRITrichopteraHydrophilidae50.0270.0510.0000.000
TRITrichopteraRhyacophilidae50.0000.0850.0000.000
TRITrichopteraUnID Trichoptera 5763.3555.0170.5220.051
TURTricladidaPlanariidae1551.3420.8810.0750.014
ZPDiplostracaCladocera30.0140.0000.0300.000
ZPHarpacticoidaCopepoda30.0140.0000.0300.000
ZPOstracodaOstracoda50.0270.0510.0000.000

References

  1. Schmidt, J.C.; Graf, J.B. Aggradation and Degradation of Alluvial Sand Deposits, 1965–1986, Colorado River, Grand Canyon National Park, Arizona; United States Geological Survey Professional Paper 1493; United States Geological Survey: Reston, VA, USA, 1990.
  2. Stevens, L.E.; Holway, J.H.; Ellsworth, C. Benthic discontinuity between an unregulated tributary and the dam-controlled Colorado River, Grand Canyon, Arizona, USA. Ann. Ecol. Environ. Sci. 2020, 4, 33–48. [Google Scholar] [CrossRef] [Scilit]
  3. Ward, J.V.; Stanford, J.A. The serial discontinuity concept of lotic ecosystems. In Dynamics of Lotic Ecosystems; Fontaine, T.D., Bartell, S.M., Eds.; Ann Arbor Science Publishers: Ann Arbor, MI, USA, 1983; pp. 29–42. [Google Scholar]
  4. Vannote, R.L.; Minshall, G.W.; Cummins, K.W.; Sedell, J.R.; Cushing, C.E. The river continuum concept. Can. J. Fish. Aquat. Sci. 1980, 37, 130–137. [Google Scholar] [CrossRef] [Scilit]
  5. Montgomery, D.R. Process domains and the river continuum. J. Am. Water Resour. Assoc. 1999, 35, 397–410. [Google Scholar] [CrossRef] [Scilit]
  6. Green, M.D.; Anderson, K.E.; Herbst, D.B.; Spasojevic, J. Rethinking biodiversity patterns and processes in stream ecosystems. Ecol. Monogr. 2022, 92, e1520. [Google Scholar] [CrossRef] [Scilit]
  7. Stevens, L.E.; Johnson, R.R.; Estes, C. Characteristics and process interactions in natural fluvial-riparian ecosystems: A synopsis of the Watershed-Continuum Model. In River Basin Management—Under a Changing Climate; Ray, R., Panagouli, D.G., Abeysingha, N., Eds.; InTechOpen: London, UK, 2022. [Google Scholar] [CrossRef] [Scilit]
  8. Strahler, A.N. Quantitative analysis of watershed geomorphology. Trans. Am. Geophys. Union 1957, 38, 913–920. [Google Scholar] [CrossRef] [Scilit]
  9. Dye, A. Contribution of Unregulated Tributaries to the Ecological Functioning of the Main Channel of Rivers. Office of Water, Sydney. 2010. Available online: https://www.researchgate.net/profile/Simon-Williams-13/publication/311427839_Contribution_of_unregulated_tributaries_to_the_ecological_functioning_of_the_main_channel_of_rivers_Snowy_Flow_Response_Monitoring_and_Modelling/links/5845f66708aeda69681a616a/Contribution-of-unregulated-tributaries-to-the-ecological-functioning-of-the-main-channel-of-rivers-Snowy-Flow-Response-Monitoring-and-Modelling.pdf (accessed on 27 January 2026).
  10. Junk, W.J.; Bayley, P.B.; Sparks, R.E. The flood pulse concept in river continuum systems. Can. Spec. Publ. Fish. Aquat. Sci. 1989, 106, 89–109. [Google Scholar]
  11. Thorp, J.; Delong, M. The riverine productivity model: An heuristic view of carbon sources and organic processing in large river ecosystems. Oikos 1994, 70, 305–308. [Google Scholar] [CrossRef] [Scilit]
  12. Hofknecht, G.W. Seasonal Community Dynamics of Aquatic Invertebrates in the Colorado River and Its Tributaries Within Grand Canyon, Arizona. Master’s Thesis, Northern Arizona University, Flagstaff, AZ, USA, 1981. [Google Scholar]
  13. Oberlin, G.E.; Shannon, J.P.; Blinn, D.W. Watershed influences on the macroinvertebrate fauna of ten major tributaries of the Colorado River through Grand Canyon, Arizona. Southwest. Nat. 1999, 44, 17–30. [Google Scholar]
  14. Blinn, D.W.; Cole, G.A. Algae and invertebrate biota in the Colorado River: Comparison of pre- and post-dam conditions. In Colorado River Ecology and Dam Management; Marzolf, G.R., Ed.; National Academy Press: Washington, DC, USA, 1991; pp. 85–104. [Google Scholar]
  15. Stevens, L.E.; Shannon, J.P.; Blinn, D.W. Benthic ecology of the Colorado River in Grand Canyon: Dam and geomorphic influences. Regul. Rivers Res. Manag. 1997, 13, 129–149. [Google Scholar] [CrossRef] [Scilit]
  16. Sublette, J.E.; Stevens, L.E.; Shannon, J.P. Chironomidae (Diptera) of the Colorado River in Grand Canyon, Arizona, USA. I: Taxonomy and ecology. Great Basin Nat. 1998, 58, 97–146. [Google Scholar]
  17. Stevens, L.E. The biogeographic significance of a large, deep canyon: Grand Canyon of the Colorado River, southwestern USA. In Global Advances in Biogeography; Stevens, L.E., Ed.; InTech Publications: Rijeka, Croatia, 2012; pp. 169–208. [Google Scholar]
  18. Cross, W.F.; Baxter, C.V.; Rosi-Marshall, E.J.; Hall, R.O., Jr.; Kennedy, T.K.; Donner, K.C.; Wellard, H.A.; Kelly, S.E.Z.; Seegert, K.E.; Behn, K.E.; et al. Food-web dynamics in a large river discontinuum. Ecol. Monogr. 2013, 83, 311–337. [Google Scholar] [CrossRef] [Scilit]
  19. Kennedy, T.A.; Muehlbauer, J.D.; Yackulic, C.B.; Lytle, D.A.; Miller, S.W.; Dibble, K.L.; Kortenhoeven, E.W.; Metcalfe, A.N.; Baxter, C.V. Flow management for hydropower exhibits aquatic insects, undermining river food webs. BioScience 2016, 66, 561–575. [Google Scholar]
  20. Abernethy, E.F.; Muehlbauer, J.D.; Kennedy, T.A.; Tonkin, J.D.; Van Driesche, R.; Lytle, D.A. Hydropeaking intensity and dam proximity limit aquatic invertebrate diversity in the Colorado River basin. Ecosphere 2021, 12, e03559. [Google Scholar] [CrossRef] [Scilit]
  21. Topping, D.J.; Schmidt, J.C.; Vierra, L.E., Jr. Computation and Analysis of the Instantaneous-Discharge Record for the Colorado River at Lees Ferry, Arizona—May 8, 1921 Through September 30, 2000; U.S. Geological Survey Professional Paper 1677; United States Geological Survey: Reston, VA, USA, 2003.
  22. Monroe, S.A.; Antweiler, R.C.; Hart, R.J.; Taylor, H.E.; Truini, M.; Rihs, J.R.; Felger, T.J. Chemical Characteristics of Ground-Water Discharge Along the South Rim of Grand Canyon in Grand Canyon National Park, Arizona, 2000–2001; U.S. Geological Survey Scientific Investigations Report 2004–5146; United States Geological Survey: Reston, VA, USA, 2005. [CrossRef] [Scilit]
  23. Wright, S.A.; Anderson, C.R.; Voichick, N. A simplified water temperature model for the Colorado River below Glen Canyon Dam. River Res. Appl. 2008, 25, 675–686. [Google Scholar] [CrossRef] [Scilit]
  24. Cooley, M.E.; Aldridge, B.N.; Euler, R.C. Effects of the Catastrophic Flood of December 1966, North Rim Area, Eastern Grand Canyon, Arizona; U.S. Geological Survey Professional Paper 980; United States Geological Survey: Reston, VA, USA, 1977. [CrossRef] [Scilit]
  25. U.S. Bureau of Reclamation. Glen Canyon Dam Long-term Experimental and Management Plan Environmental Impact Statement. U.S. Department of the Interior, Washington. 2016. Available online: https://ltempeis.anl.gov/documents/final-eis/ (accessed on 27 January 2026).
  26. Webb, R.H.; Pringle, P.T.; Rink, G.R. Debris Flows from Tributaries of the Colorado River, Grand Canyon National Park, Arizona; U.S. Geological Survey Professional Paper 1492; United States Geological Survey: Reston, VA, USA, 1989.
  27. Melis, T.S.; Webb, R.H.; Griffiths, P.G. Debris flows in Grand Canyon National Park: Peak discharges, flow transformations, and hydrographs. In Debris-Flow Hazards Mitigation: Mechanics, Prediction, and Assessment; Chen, C.-L., Ed.; American Society of Civil Engineers: New York, NY, USA, 1997; pp. 727–736. [Google Scholar]
  28. Webb, R.H.; Griffiths, P.G.; Melis, T.S.; Hartley, D.R. Sediment Delivery by Ungagged Tributaries of the Colorado River in Grand Canyon, Arizona; U.S. Geological Survey Water-Resources Investigations Report 00-4055; United States Geological Survey: Reston, VA, USA, 2000.
  29. Woodbury, A.M. (Ed.) Ecological Studies of the Flora and Fauna in Glen Canyon; University of Utah Anthropological Papers; University of Utah Press: Salt Lake City, UT, USA, 1959; Volume 40, pp. 1–229. [Google Scholar]
  30. Webb, R.H. Grand Canyon, A Century of Change: Rephotography of the 1889–1890 Stanton Expedition; University of Arizona Press: Tucson, AZ, USA, 1996. [Google Scholar]
  31. Tobin, B.W.; Springer, A.E.; Kreamer, D.K.; Schenk, E.R. Review: The distribution, flow, and quality of Grand Canyon springs, Arizona (USA). Hydrogeol. J. 2017, 26, 721–732. [Google Scholar] [CrossRef] [Scilit]
  32. Crossey, L.; Fischer, T.P.; Patchett, P.J.; Karlstrom, K.E.; Hilton, D.R.; Newell, D.; Huntoon, P.; Reynolds, A.C.; De Leeuw, G.A. Dissected hydrologic system at the Grand Canyon: Interaction between deeply derived fluids and plateau aquifer waters in modern springs and travertine. Geology 2006, 34, 25. [Google Scholar] [CrossRef] [Scilit]
  33. Unema, J.A.; Anderson, J.R.; Chapin, T.P.; Tillman, F.D. Water Quality Data from Select Spring and Stream Sites and Water and Sediment Quality Data from the Colorado River and Major Tributaries in Grand Canyon, Northern ARIZONA (Ver. 2.0, April 2024); U.S. Geological Survey Data Release; United States Geological Survey: Reston, VA, USA, 2020. [CrossRef]
  34. Merritt, R.W.; Cummins, K.W.; Berg, M.B. An Introduction to the Aquatic Insects of North America, 4th ed; Kendall-Hunt Publishing Company: Dubuque, Iowa, USA, 2008. [Google Scholar]
  35. Sabo, J.L.; Post, D.M. Quantifying periodic, stochastic, and catastrophic environmental variation. Ecol. Monogr. 2008, 192, 19–40. [Google Scholar] [CrossRef] [Scilit]
  36. Sabo, J.L.; Ruhi, A.; Holtgrieve, G.W.; Elliott, V.; Arias, M.E.; Ngor, P.B.; Räsänen, T.A.; Nam, S. Designing river flows to improve food security futures in the Lower Mekong Basin. Science 2017, 358, eaao1053. [Google Scholar] [CrossRef] [Scilit]
  37. Deng, Q.; Sabo, J.L.; Holtgrieve, G.W.; Ngor, P.B.; Holway, J. Timing of hydrologic anomalies direct impacts on migration traits in a flood pulse fishery system. J. Appl. Ecol. 2023, 60, 494–506. [Google Scholar] [CrossRef] [Scilit]
  38. Platts, W.S.; Meghan, W.F.; Minshall, G.W. Methods for Evaluating Stream Riparian and Biotic Conditions. U.S. Department of Agriculture Forest Service General Technical Report INT-1983, Ogden; 1983. Available online: https://research.fs.usda.gov/treesearch/29138 (accessed on 27 January 2026).
  39. Connell, J.H. Diversity in tropical rain forests and coral reefs. Science 1979, 199, 1302–1310. [Google Scholar]
  40. Huston, M.A. A general hypothesis of species diversity. Am. Nat. 1979, 113, 81–101. [Google Scholar] [CrossRef] [Scilit]
  41. Huston, M.A. Biological Diversity: The Coexistence of Species on Changing Landscapes; Cambridge University Press: Cambridge, UK, 1994. [Google Scholar]
  42. Rundio, D.E. Community-habitat relationships in coastal streams in Big Sur, California, USA: Travertine influences macroinvertebrate abundance and community structure. Hydrobiologia 2009, 620, 91–108. [Google Scholar] [CrossRef] [Scilit]
  43. Sada, D.W.; Thomas, J.M. Relationships between aquatic ecology, landscapes, hydrogeology and hydrogeochemistry in Great Basin and Mojave Desert spring ecosystems USA. Ecohydrology 2025, 18, 370035. [Google Scholar] [CrossRef] [Scilit]
  44. Yard, M.D.; Bennett, G.E.; Mietz, S.N.; Coggins, L.G., Jr.; Stevens, L.E.; Hueftle, S.; Blinn, D.W. Influence of topographic complexity on solar insolation estimates for the Colorado River, Grand Canyon, AZ. Ecol. Model. 2005, 183, 157–172. [Google Scholar] [CrossRef] [Scilit]
  45. Protiva, F.R.; Ralston, B.E.; Stone, D.M.; Kohl, K.A.; Yard, M.D.; Haden, G.A. Effects of Glen Canyon Dam Discharges on Water Velocity and Temperatures at the Confluence of the Colorado and Little Colorado Rivers and Implications for Habitat for Young-of-Year Humpback Chub (Gila cypha); U.S. Geological Survey Open-file Report 2010-1137; United States Geological Survey: Reston, VA, USA, 2010.
  46. Minshall, G.W. Responses of stream benthic macroinvertebrates to fire. For. Ecol. Manag. 2003, 178, 155–161. [Google Scholar] [CrossRef] [Scilit]
Figure 1. Schematic confluence of a tributary with a mainstream river. Tributary characteristics and processes can differ greatly from those of the mainstream, depending on the relative magnitude of differences in each stream’s characteristics. Habitats include the following: A—tributary away from mainstream influences; B—confluence zone (mouth); C—the mainstream not influenced by the tributary.
Water 18 00395 g001
Figure 2. A conceptual model of the magnitude of AMI discontinuity in relation to differences in mainstream embeddedness of firm substrata in fine sand versus tributary-based geochemical carbonate cementation of the channel floor. Either process can occur in a tributary or a mainstream, with gradient interaction additively limiting AMI assemblage complexity. S hat—expected AMI assemblage species richness; D hat—expected AMI density/m2.
Water 18 00395 g002
Figure 4. Water-quality variation among tributary, confluence zone (mouth), and mainstream Colorado River habitats: (a) mean water temperature (°C); (b) pH; (c) specific conductance (μS/cm2). Error bars are 95% confidence intervals.
Water 18 00395 g004
Figure 5. Aquatic macroinvertebrate sampling data: (a) mean species richness/sample (S); (b) mean density of individuals/m2; (c) mean Ephemeroptera + Plecoptera + Trichoptera (EPT) species richness/sample; and (d) mean EPT density/m2. Error bars are 95% confidence intervals.
Water 18 00395 g005
Figure 6. CCA biplots showing the responses of AMI composition and density/m2 in relation to (a) hydrologic regime and (b) embeddedness in relation to substratum grain size. IDI—days between low-flow events; IFI—inter-flood interval; MaxHSAM—maximum highest spectral anomaly magnitude; RangeNAA—range of net annual (discharge) anomaly; substrata—silt (<0.05 mm), sand, fine gravel (F Gvl 0.1–1 cm), coarse gravel (C Gvl, 1–10 cm), small boulders, (S Bdr, <1 m), large boulder (L Bddr, >1 m), bedrock (Bdrk); Velocity (m/s). AMI taxon abbreviations are listed in Appendix A.
Water 18 00395 g006
Figure 7. Dmag as a function of sampling site distance (km) downstream from Glen Canyon Dam through Grand Canyon. Fourth-order polynomial R2 = 0.631. High values in the middle and lowermost Grand Canyon were related to low specific conductance of springs emerging from karstic aquifers.
Water 18 00395 g007
Figure 8. Mean aquatic macroinvertebrate density/m2 sampled from 24 tributaries and the adjacent mainstream in Grand Canyon in relation to low-to-high observations of the extent of carbonate cementation of channel floors and embeddedness of benthic substrata in fine sand. Numbers within cells are mean AMI species richness over mean density/m2. AMI taxon abbreviations are listed in Appendix A.
Water 18 00395 g008
Figure 9. Pre-dam aquatic insect species richness in three habitats in the Colorado River basin in Glen Canyon, Utah (data from Woodbury [29]). Sample size: 33 tributaries, 12 confluence zones (tributary mouths); 7 mainstream river sites; error bars are 95% confidence intervals.
Water 18 00395 g009
Table 1. Relative levels of embeddedness and cementation, velocity (m/s), field water quality, and tributary-to-mainstream discontinuity magnitude (Dmag) of the confluence zone (mouth), mainstream, and tributary upstream from mainstream impacts, mean number of AMI species/sample, mean density/m2 by tributary (planview basin area, km2, [27]) and distance downstream from Lees Ferry (Rkm), Colorado River in Grand Canyon, Arizona. Site numbers refer to map locations in Figure 3.
Tributary (Basin Area km2)RkmHabitatRelative Embed-dednessRelative Cement-ationV (m/s)Temp. °CpHSpecific Cond (μS/cm)Mean No. Species/
Sample
Mean No. Individs/
m2)
Dmag
1. Paria River (3670)2MouthHighlow0.0123.88.088133.67.2−0.316
RiverHighlow0.3518.27.7067064.52150.5
TribMedhigh0.12208.6052869.6310.5
2. Vaseys Paradise (0.5)51MouthLowlow2.00178.30316108.512,899.2−0.077
RiverHighlow1.3318.37.80670138.92037.0
3. Saddle Canyon (29.3)76RiverHighlow2.6718.37.80670139.91766.80.211
TribLowhigh0.11268.64434107.42233.6
4. Nankoweap Creek (84.6)84MouthLowhigh0.4421.77.80670104.2437.5−0.196
RiverHighlow0.0718.57.80670170.51356.6
TribLowhigh0.34287.8067092.6629.6
5. Little Colorado River (69,000)98MouthHighmed0.27228.1 439628.771.8−0.286
RiverHighlow0.1118.97.8067035.9563.3
TribMedhigh0.76258.1 439625.139.5
6. Chuar Creek (54.7)105MouthHighhigh0.20---7.1316,9630.00.0−1.000
RiverHighlow0.1017.48.2092021.321.3
TribMedhigh0.10---7.1316,9630.00.0
7. Clear Creek (93.1)135MouthLowmed0.40259.00340255.81427.60.317
RiverHighlow0.2519.18.1059896.9164.9
TribLowmed0.0832.19.00340115.1676.0
8. Bright Angel Creek (260.3)142MouthLowmed0.5419.98.7033586.1355.20.880
RiverHighlow0.2619.28.1059517.950.2
TribLowlow0.2619.98.70335153.51289.3
9. Pipe Creek (17.3)143MouthMedlow1.6021.18.6238586.1599.20.800
RiverHighlow0.7319.08.2059325.135.9
TribLowlow0.9521.18.60385100.51905.3
10. Hermit Creek (32.0)153MouthLowlow0.4323.48.3868984.4276.30.636
RiverHighlow1.0013.58.0183561.4583.3
TribLowmed0.3023.86.58681138.1260.9
11. Boucher Creek (16.8)156MouthMedlow0.1119.58.301097229.45623.70.276
RiverHighlow0.1119.68.1059766.175.4
TribLowmed0.2830.18.301097189.4927.4
12. Crystal Creek (111.6)158MouthMedlow0.7527.38.80707111.11888.90.651
RiverHighlow0.5019.98.2059455.6703.7
TribLowhigh0.5927.38.80707126.2457.8
13. Shinumo Creek174RiverLowlow0.1017.48.6092010.613.80.900
TribLowlow0.3021.48.20329106.4350.0
14. Royal Arch Creek (30.9)187MouthMedlow0.8322.18.3089117.971.70.811
RiverHighlow0.7320.18.2059539.468.1
TribLowlow0.5724.28.30891143.45190.0
15. Stone Creek (6.8)212MouthLowmed0.4222.88.7645143.0236.20.667
RiverHighlow0.3320.28.3183323.07.7
TribLowlow0.80238.49448115.192.9
16. Tapeats Creek (216.3)216MouthLowlow0.4715.18.2032899.81650.00.778
RiverHighlow0.6219.88.2061874.1870.4
TribLowlow1.4015.18.20328222.26018.5
17. Deer Creek (43.6)219MouthMedlow0.0820.38.6039335.8405.00.742
RiverHighlow0.5720.38.2061364.8213.0
TribLowlow1.4219.58.6039391.41494.2
18. Kanab Creek (6382)232MouthHighlow0.0025.68.50115838.499.80.525
RiverHighlow0.0720.48.2060223.046.0
TribMedmed0.5125.68.50115837.0268.5
19. Matkatamiba Creek (80.8)235MouthMedlow0.2025.58.76143435.8379.90.552
RiverHighlow0.7317.38.4482521.543.0
TribLowlow0.2322.67.73143660.91476.7
20. Havasu Creek (7800)253MouthHighmed0.1722.18.4169025.150.20.667
RiverHighlow0.1017.38.4482510.610.6
TribMedhigh0.8022.18.4169064.5168.5
21. Spring (0.1)265TribLowlow0.2731.48.61195521.525.10.714
RiverHighlow0.1520.68.146123.63.6
22. Spring Creek (50.4)328MouthHighlow0.1726.78.106140.00.0−1.000
RiverHighlow0.1220.48.0059618.5240.7
23. Pumpkin Spring (0.1)341TribHighmed0.0533.26.3014,6010.00.0−1.000
RiverHighlow0.0520.48.0059627.8202.8
24. Surprise Canyon (423)399MouthHighmed0.20257.6992442.641.50.800
RiverHighlow0.22198.3889321.342.6
TribMedhigh0.16257.60924138.3710.6
Table 2. Numbers of sites with levels of embeddedness and cementation among tributary, confluence zone (mouth), and mainstream Colorado River habitats sampled in Grand Canyon. Not all tributaries reached the mainstream, resulting in unequal totals/habitat.
Cementation
HabitatEmbeddedLowMedHighTotal
TributaryLow93315
Med0156
High0101
MouthLow3317
Med6006
High3317
RiverLow1001
Med0000
High230023
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.