
Article

Invasion Status, Distribution, and Environmental Preferences of Non-Native Ornamental Thunbergia Species (Acanthaceae) in Ecuador: An Emerging Threat to Tropical Montane Forests

1
Escuela de Ciencias Ambientales, Universidad Espíritu Santo (UEES), Samborondón 091650, Ecuador
2
Instituto Nacional de Biodiversidad (INABIO), Quito 170105, Ecuador
3
Departamento de Ciencias Ecológicas, Facultad de Ciencias, Universidad de Chile, Santiago 8320000, Chile
4
Instituto de Ecología y Biodiversidad (IEB), Santiago 8320000, Chile
5
Centro de Investigación de la Biodiversidad y Cambio Climático (BioCamb), Facultad de Ciencias de Medio Ambiente, Universidad Tecnológica Indoamérica, Quito 170301, Ecuador
6
Botanic Institute of Barcelona (IBB), CSIC-CMCNB, 08038 Barcelona, Catalonia, Spain
*
Authors to whom correspondence should be addressed.
Forests 2026, 17(3), 363; https://doi.org/10.3390/f17030363
Submission received: 4 February 2026 / Revised: 3 March 2026 / Accepted: 11 March 2026 / Published: 14 March 2026
(This article belongs to the Special Issue Non-Native Species in Forest Ecosystems)

Abstract

Species of the genus Thunbergia, native to Africa, Asia, and Australia, are widely cultivated as ornamental plants; however, their ability to escape cultivation and establish themselves in novel environments poses a growing threat to tropical forests. Here, we provide the first nationwide assessment of Thunbergia species occurring in Ecuador, integrating data from citizen science platforms, herbarium collections, and field surveys. We analyzed spatiotemporal patterns of occurrence, evaluated invasion status based on wild persistence and spread, and assessed environmental preferences using climatic niche analyses. Species distributions were further examined across land-cover types, conservation areas, and forest–non-forest interfaces. We confirmed the presence of five Thunbergia species in Ecuador, two of which also occur in the Galapagos Islands. All species were recorded both in cultivation and in the wild, indicating ornamental horticulture as the main introduction pathway for the genus, and occurrences were documented within 24 conservation areas. Thunbergia alata, T. fragrans, and T. grandiflora were categorized as invasive in Ecuador. Among them, T. fragrans exhibited broad environmental tolerance across bioregions. Wild occurrences were predominantly associated with human-modified landscapes but frequently occurred near forest edges, indicating ongoing encroachment into natural forests. These findings highlight the urgent need for preventive and targeted management strategies, particularly against T. alata, which represents an emerging threat to Andean forest ecosystems.

1. Introduction

A large proportion of the plants that compose urban ecosystems are non-native species cultivated by people, mostly for ornamental purposes [1]. Urban habitats are well documented as hotspots for the establishment and spread of non-native plants due to high colonization and propagule pressures driven by trade, transportation, frequent and intense disturbances, and, in particular, horticultural activities [2]. Moreover, a substantial proportion of naturalized and invasive alien plants are cultivated in domestic and botanical gardens or commercialized as ornamentals [3,4], highlighting the disproportionate influence of ornamental trade and cultivation practices on the global establishment of non-native species. Additionally, the process of domestication and horticultural breeding—aimed at traits such as rapid growth, tolerance to a wide range of environmental conditions, profuse reproduction, and prolonged flowering—often inadvertently selects for characteristics associated with invasiveness [4,5].
Intentional introductions through ornamental horticulture represent the largest pathway for the global spread of invasive alien plant species. At the global scale, ornamental taxa account for approximately 40%–80% of alien plants that have become naturalized or invasive [6]. Africa, Asia-Pacific, Europe, North America, and West Asia follow this pattern; Latin America and the Caribbean also show similar trends, with nearly 40% of invasive plant species introduced for ornamental purposes [3]. In Brazil, 62% of non-native invasive plant species (201 species) are reported to have ornamental use [7]. In Mexico, the main introduction pathway for alien vascular plants is ornamental horticulture, mainly through garden escapes and the nursery trade [8]. Likewise, across Central America, most alien plant species (about 60%) were intentionally introduced for ornamental purposes [9].
In Ecuador, horticulture also represents a major pathway for the introduction of non-native plants, mirroring global patterns. A recent national catalog of non-native vascular flora documented 1260 alien taxa for continental Ecuador, of which 486 occur in the wild; notably, ornamental use is the most frequent among them, accounting for 42% of the wild taxa [10]. The Andean region harbors the highest richness of non-native plants, including ornamentals, likely due to its dense human population, historical trade routes, and high levels of habitat disturbance [10]. Despite the ecological relevance of ornamentals in Ecuador’s non-native flora, no national blacklists or internal trade restrictions currently exist for invasive ornamentals, meaning that many species with recognized invasive potential remain freely available in horticultural markets and gardens. This regulatory gap, coupled with ongoing introductions and insufficient systematic monitoring, underscores the urgent need for targeted prevention and management strategies in the country.
The introduction of ornamental plants into urban and peri-urban environments often represents the first step in their escape and subsequent naturalization in surrounding natural habitats [11,12,13]. In tropical countries like Ecuador, where urban areas are closely connected to montane and forest ecosystems, horticultural species can easily spread beyond cultivation. Major cities like Quito and Cuenca are embedded within the Andean region and directly border cloud forests, montane forests, or páramo ecosystems (e.g., [14]). In Amazonian cities like Tena or Puyo, urban settlements are surrounded by tropical rainforests with little or no buffer zone. This transition from garden to wild landscapes appears to be the case for several species of the genus Thunbergia that have escaped from cultivation.
Thunbergia, clockvines, is a genus of shrubs and climbing vines in the family Acanthaceae, native to tropical and subtropical regions of Africa, Asia, and Australia [15]. Its species produce large, showy flowers that bloom year-round, attract a variety of pollinators, and are widely used in landscaping and gardening as ornamental shrubs or climbers [16]. Due to their ornamental value, several Thunbergia species have been introduced beyond their native range and have become environmental threats by escaping cultivation in the Neotropics (e.g., [17,18,19]) and the tropical Indo-Pacific islands [20]. Functional traits documented in different Thunbergia species may contribute to their invasiveness in tropical forests. In T. alata, morphological and anatomical adaptations as well as strong associations with arbuscular mycorrhizal fungi have been reported [21], and physiological seed dormancy may further enhance persistence and recruitment [22]. In T. grandiflora, tolerance to high light conditions and acidic soils has been documented, supporting its establishment in disturbed habitats [21,22,23]. When invasive, some Thunbergia species spread rapidly by overgrowing host trees and forming dense understory mats, thereby smothering native vegetation, increasing tree fall, and limiting seed germination and seedling establishment [20,24,25,26,27]. In the Central Andes of Colombia, Thunbergia alata is listed among the ten most problematic invasive species [28]. Its rapid colonization and successful adaptation in Colombian Andean forests have led to the development of targeted management strategies [21]. In continental Ecuador, four Thunbergia species have been reported to be growing in the wild to date (T. alata, T. erecta, T. fragrans, and T. grandiflora) [10], whereas only T. erecta and T. fragrans occur in the Galapagos Islands [29]. Populations of the vine T. alata in the Ecuadorian Andes—mainly around the city of Quito—have been subject to control efforts due to their dense proliferation in forests, which causes tree mortality [30]. Despite the potential ecological impacts of Thunbergia species in Ecuadorian forests—particularly those of the Andean region—and in the Galapagos Islands, no comprehensive nationwide assessments of these taxa have been undertaken so far.
To address these knowledge gaps, we combined comprehensive occurrence data with spatial, temporal, and environmental analyses to produce the first nationwide assessment of Thunbergia in Ecuador. Specifically, we aimed to (1) provide an updated and reliable list of both wild and cultivated Thunbergia species in Ecuador—including the Galapagos Islands, along with an identification key; (2) examine the temporal accumulation and spatial distribution of all records by species; (3) characterize the environmental preferences of the species occurring in the wild; (4) estimate their invasion status (i.e., casual, naturalized, or invasive) across land-cover types, within conservation areas, and at the national scale. Through this integrated approach, our study delivers a comprehensive baseline to support early detection, monitoring, and management planning.

2. Materials and Methods

2.1. Study Area

This study encompasses both continental Ecuador and the Galapagos Islands. Continental Ecuador is located in northwestern South America, bordered by Colombia, Peru, and the Pacific Ocean, while the Galapagos, a volcanic archipelago, lie ca. 1000 km offshore. The country comprises four bioregions: three that correspond to the mainland (Coastal, Andean, Amazonian) and one that exactly matches the Galapagos Islands (the Insular bioregion) [31], covering about 283,000 km2 in total [32]. The coastal bioregion includes humid and dry forests, shrublands, and mangroves, with temperatures of 24–25 °C and rainfall from 60 to 2000 mm/year [33,34]. The Andean bioregion mainly hosts montane forests and páramos, with temperatures of 8–20 °C and 800–1500 mm of precipitation per year [31,35]. The Amazonian bioregion features lowland rainforests, with average temperatures of 24–25 °C and over 4500 mm of annual rainfall [36]. The Galapagos Islands have an arid lowland and humid highland climate, with a mean temperature of 23 °C [31].
Ecuador is one of the world’s 17 megadiverse countries [37], with ca. 18,200 vascular plant species, including about 4500 endemics [32,38]. It hosts a broad network of conservation areas, including 79 protected areas that are part of the National System of Protected Areas (SNAP in its Spanish acronym)—which comprises both state-managed and privately managed reserves—and 175 Areas of Forest and Protective Vegetation (ABVP in its Spanish acronym) [39]. Despite this exceptional biodiversity, biological invasions pose increasing threats, especially in the Galapagos Islands, where isolation and high vulnerability lead to substantial management costs [40].

2.2. Data Sources and Curation of Thunbergia Records

To generate an updated list of Thunbergia species in Ecuador, we carried out a comprehensive compilation of occurrence data available up to December 2024, integrating multiple sources: (i) specimens from the national Herbaria (HA, QCA, and QCNE) were examined directly in herbarium collections, while additional specimens from national (CDS, CHEP, and ECUAMZ) and international (AAU, FLAS, MO, NY, RB, S, US, and USF) herbaria were accessed through digital repositories (see Supplementary Materials, Table S1); (ii) national and global biodiversity databases, including the Catalog of the Vascular Plants of Ecuador (W3CEC) (http://legacy.tropicos.org/Project/CE; accessed on 2 May 2024) and the Global Biodiversity Information Facility (GBIF; https://doi.org/10.15468/dl.5nuwc5; accessed on 2 May 2024); (iii) citizen science platforms, including iNaturalist (https://www.inaturalist.org/; accessed on 9 January 2025), Observation.org (https://observation.org/; accessed on 9 January 2025), and PlantNet (https://plantnet.org/en/; accessed on 9 January 2025). In addition, we incorporated personal field observations conducted between 2023 and 2024, which were uploaded to iNaturalist to complement the occurrence dataset. No new voucher specimens were collected or deposited in herbaria specifically for this study. A structured database was developed for all records, capturing the following information: record type, source, ID or specimen code, collector or observer, year of collection or observation, locality description, species name, geographic coordinates, and coordinate accuracy.
All records were manually reviewed and curated. We retained only those that had been directly observed—either in the field or verified through herbarium specimens—or that were supported by photographic evidence. Each entry was evaluated to confirm its taxonomic identity, and misidentified specimens were corrected where possible based on morphological traits. Records were excluded if they had uncertain identifications, lacked date information, or showed inconsistencies between geographic coordinates and locality descriptions. A single record without geographic coordinates, corresponding to the oldest known record of Thunbergia fragrans, was included in the dataset but excluded from the analysis.
Because a substantial proportion of the dataset originated from citizen science platforms, particular attention was given to data reliability. All citizen science records were independently reviewed by the authors through detailed examination of photographic evidence and associated metadata to confirm taxonomic identity and record status. In addition, targeted field visits were conducted to validate selected populations and doubtful observations contributed by other users. Records lacking sufficient diagnostic information were excluded.
The taxa list was further screened for taxonomic name standardization using the World Checklist of Vascular Plants (WCVP; [41]). To support accurate species identification, a dichotomous key was developed based on reliable morphological characters observed in herbarium specimens, field photographs, and existing floristic treatments.

2.3. Spatio-Temporal Patterns of Records

For each species, we documented the year and locality of the earliest record. For all species except T. mysorensis, this information was obtained from preserved herbarium specimens deposited in several national and international herbaria. For T. mysorensis, it was derived from observational records due to the absence of herbarium material. The temporal dynamics of Thunbergia records were analyzed using species-specific accumulation curves, which represent the cumulative number of records per species over time (years). Additionally, spatio-temporal maps were generated for each Thunbergia species to illustrate changes in geographic distribution over time. Records were grouped into four intervals (≤1985, ≤1998, ≤2011, ≤2024) and plotted to show the cumulative expansion of each species across continental Ecuador and the Galapagos Islands.

2.4. Invasion Status

To categorize Thunbergia species according to their invasion status, records were classified into three categories: (i) wild occurrences, (ii) cultivated occurrences, and (iii) uncertain occurrences (when it could not be determined whether the record represented cultivation or wild growth). For herbarium specimens, classification was derived directly from the information provided on the specimen label. Records were assigned to the cultivated category when the label explicitly indicated cultivation, and to the wild category when the label specified that the species occurred in natural or unmanaged conditions. Specimens lacking explicit information on origin or status were classified as uncertain. For records obtained from iNaturalist observations, we reviewed both the notes provided by observers and the accompanying photographs to verify taxonomic identity and record status, following the validation approach described by Vargas et al. [42]. This manual verification was necessary because users frequently omit selecting the “cultivated” option on the platform [43]. When the photographs clearly indicated that the plant was cultivated—for example, growing in a garden or in a pot—the record was classified as cultivated. Conversely, when images showed the species occurring under natural or unmanaged conditions, records were assigned to the wild category. In cases where the photographic evidence suggested that the observer may have omitted selecting the “cultivated” option during upload, we contacted the corresponding iNaturalist user to confirm the status of the record. When neither the annotations nor the photographs provided sufficient information, and when the contacted observer could not recall the conditions of the observation, the record was classified as uncertain.
To ensure a precise correspondence between invasion status and geographic location, we only included records with a spatial uncertainty of less than 1 km. Wild occurrences were further classified into four categories: (i) casual, (ii) naturalized, (iii) invasive, and (iv) uncertain. Casual occurrences refer to one or several individuals that cannot be assumed to have formed a self-replacing population. Naturalized occurrences include several individuals that have persisted over time in unmanaged areas or that occupy a broad extent without apparent impacts on the native vegetation. For these records, we evaluated whether the same locality had documented the species in previous years, which would indicate population persistence at the site and thus suggest its establishment. Invasive occurrences are characterized by populations occupying extensive areas, often covering large portions of the habitat and causing impacts on native vegetation, crops, or infrastructure. For practical reasons, the assignment of records to these three categories does not strictly follow the classical criteria of [44], but it also incorporates additional criteria that can be useful for inferring invasion status, particularly when photographs are used. These supplementary criteria include measures of abundance or dominance [45] and evidence of impacts on vegetation or the surrounding environment (see [46] for a discussion on the issue). Uncertain occurrences refer to records that were confirmed to be in wild conditions but lacked sufficient evidence to be confidently assigned as casual, naturalized, or invasive. This was common for herbarium specimens labeled as occurring in natural areas without details on abundance or cover, as well as for citizen science observations where the location indicated a natural habitat, but the photographs did not provide enough information to determine population extent or cover.

2.5. Environmental Preferences

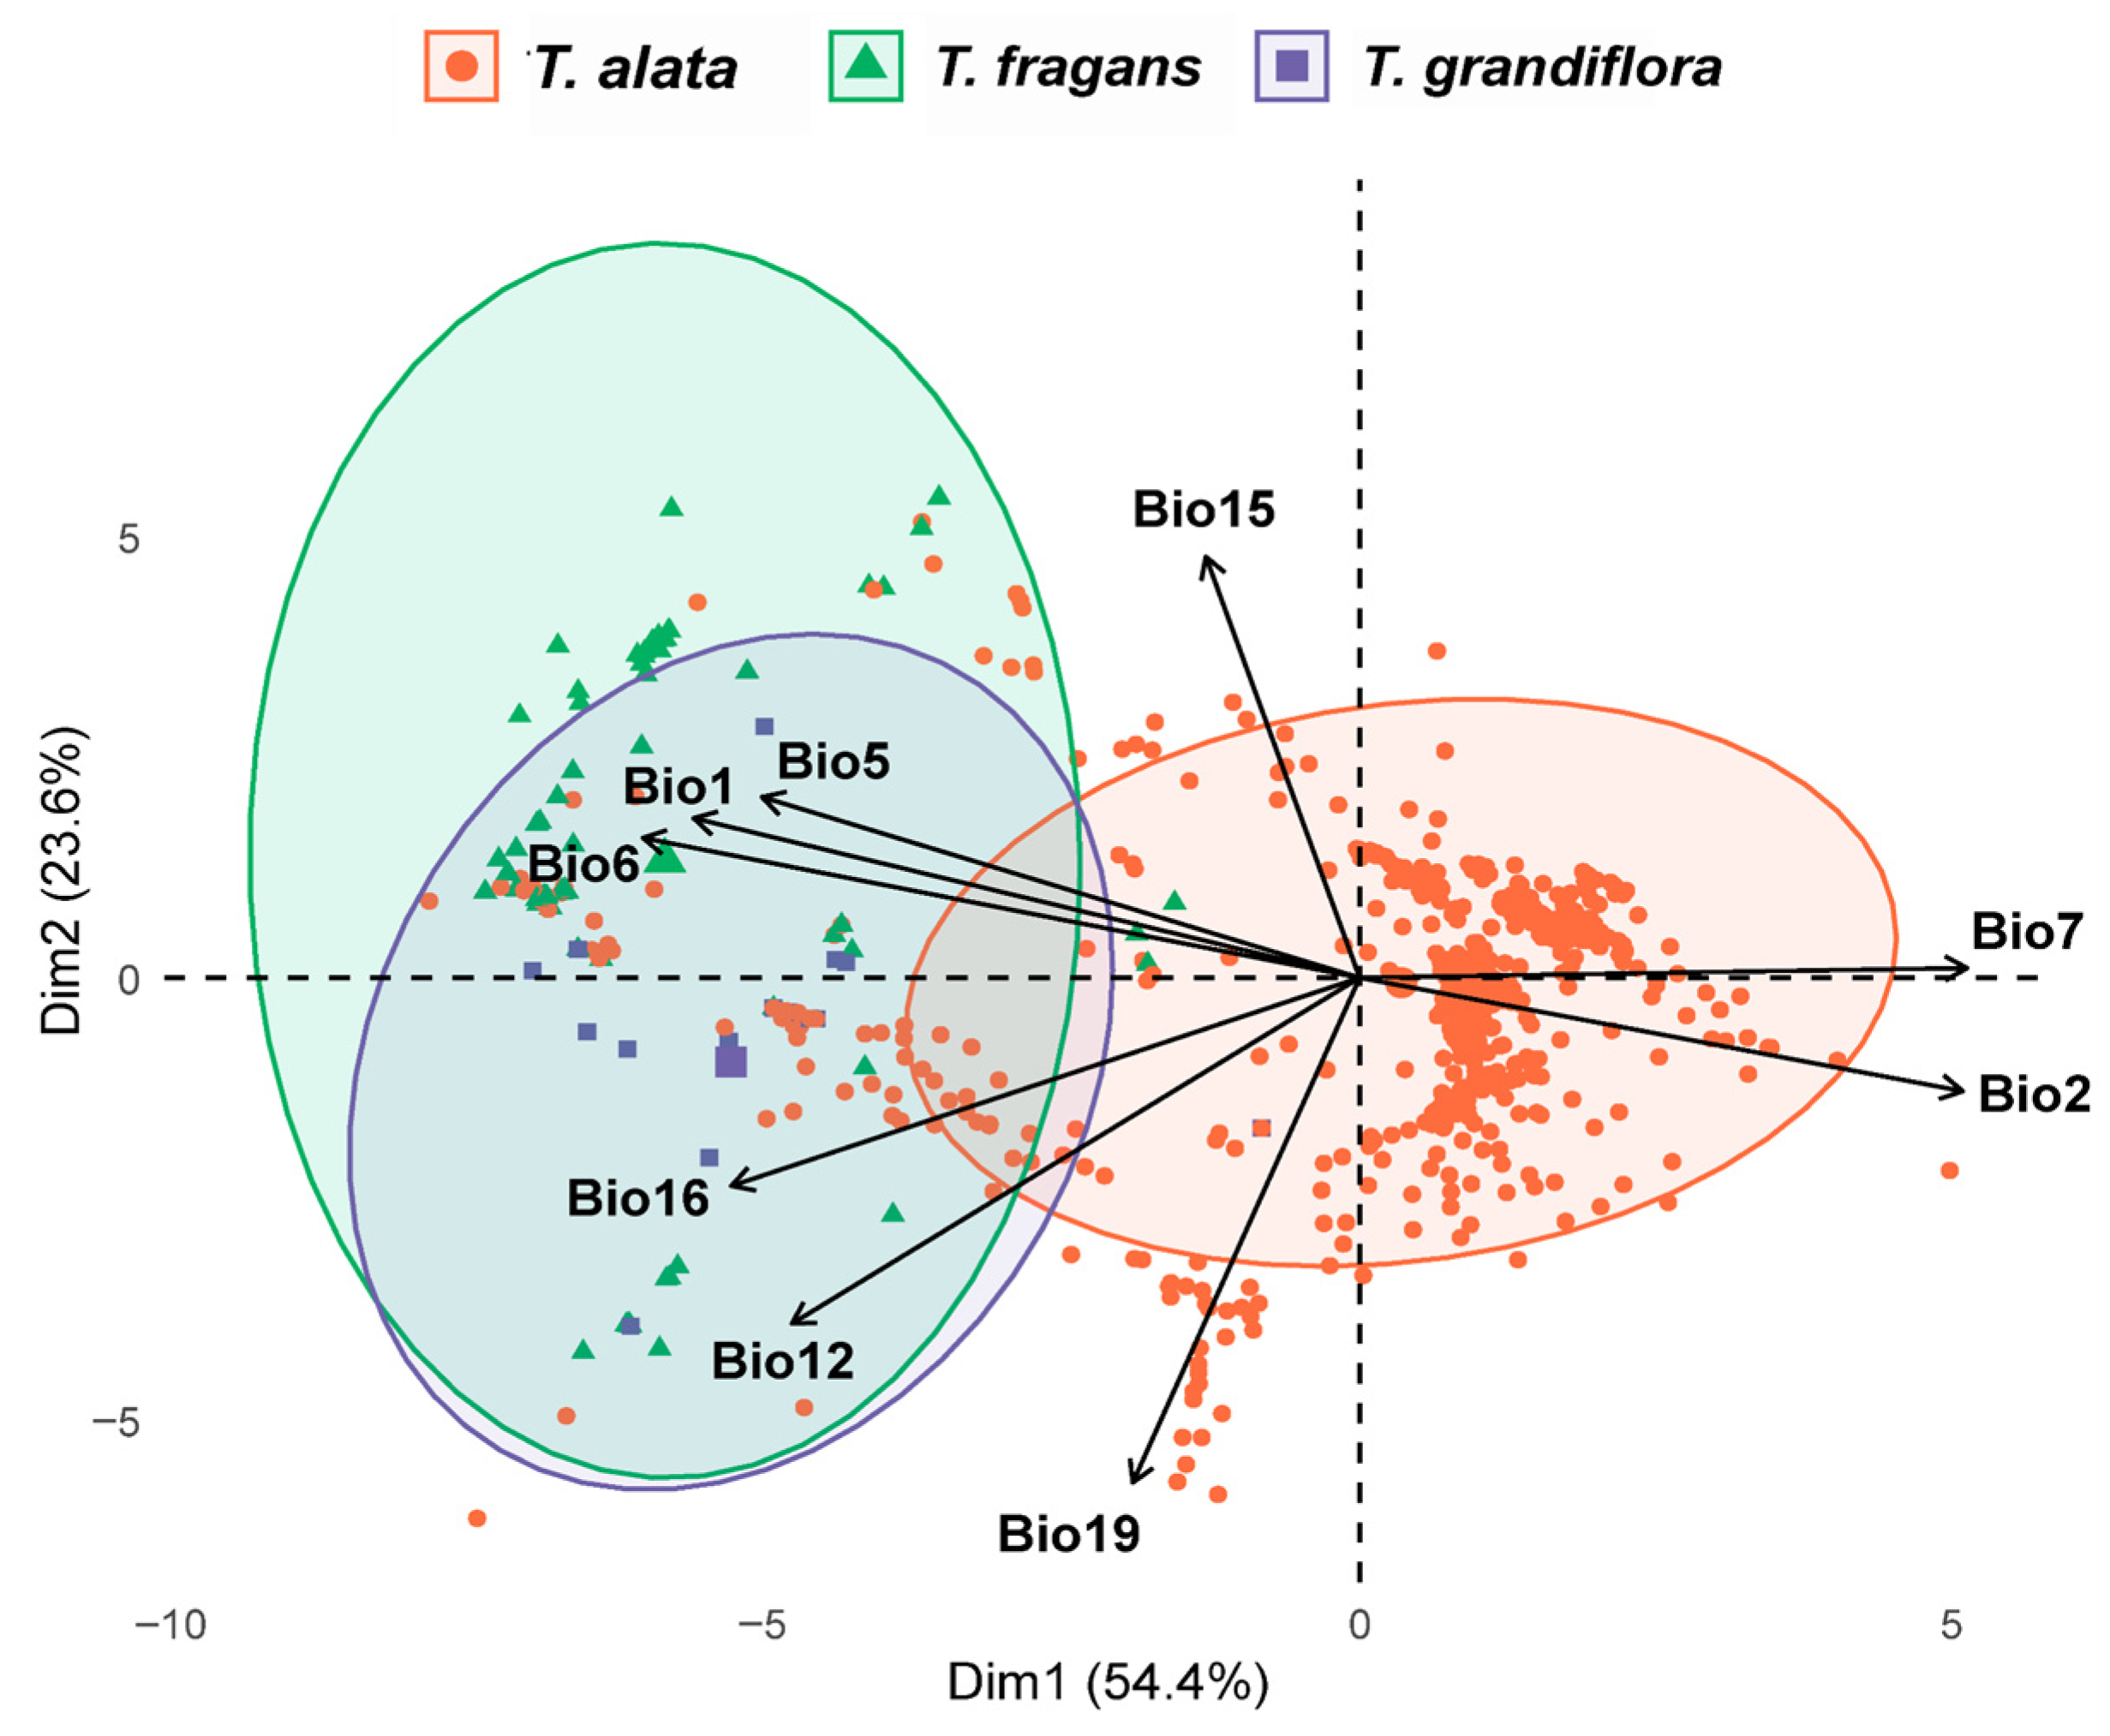
To characterize the environmental conditions associated with wild records of Thunbergia species in Ecuador, bioclimatic variables were obtained from the CHELSA database (Climatologies at High Resolution for the Earth’s Land Surface Areas; https://www.chelsa-climate.org/; accessed on 21 May 2025). The analysis included only georeferenced wild occurrences with a spatial precision buffer ≤1 km. Due to the limited number of records, T. mysorensis and T. erecta were excluded. Climate variable extraction and processing were conducted in RStudio v. 4.5.1 [47]. To select the climatic variables, we performed a Principal Component Analysis (PCA) using the 19 bioclimatic variables in R (https://www.r-project.org/) with the package ecospat [48]. Based on the correlation matrix derived from the PCA, we selected variables that were weakly correlated (Spearman’s r < |0.7|) and of ecological relevance to the studied species. The final set included nine bioclimatic variables: annual mean temperature (BIO1), mean diurnal temperature range (BIO2), maximum temperature of the warmest month (BIO5), minimum temperature of the coldest month (BIO6), temperature annual range (BIO7), annual precipitation (BIO12), precipitation seasonality (BIO15), precipitation of the wettest quarter (BIO16), and precipitation of the coldest quarter (BIO19). After selecting these variables, we performed a final PCA and frequency histograms of occurrence were generated for each variable by species.

2.6. Invasion Status Across Land-Cover Types and Conservation Areas

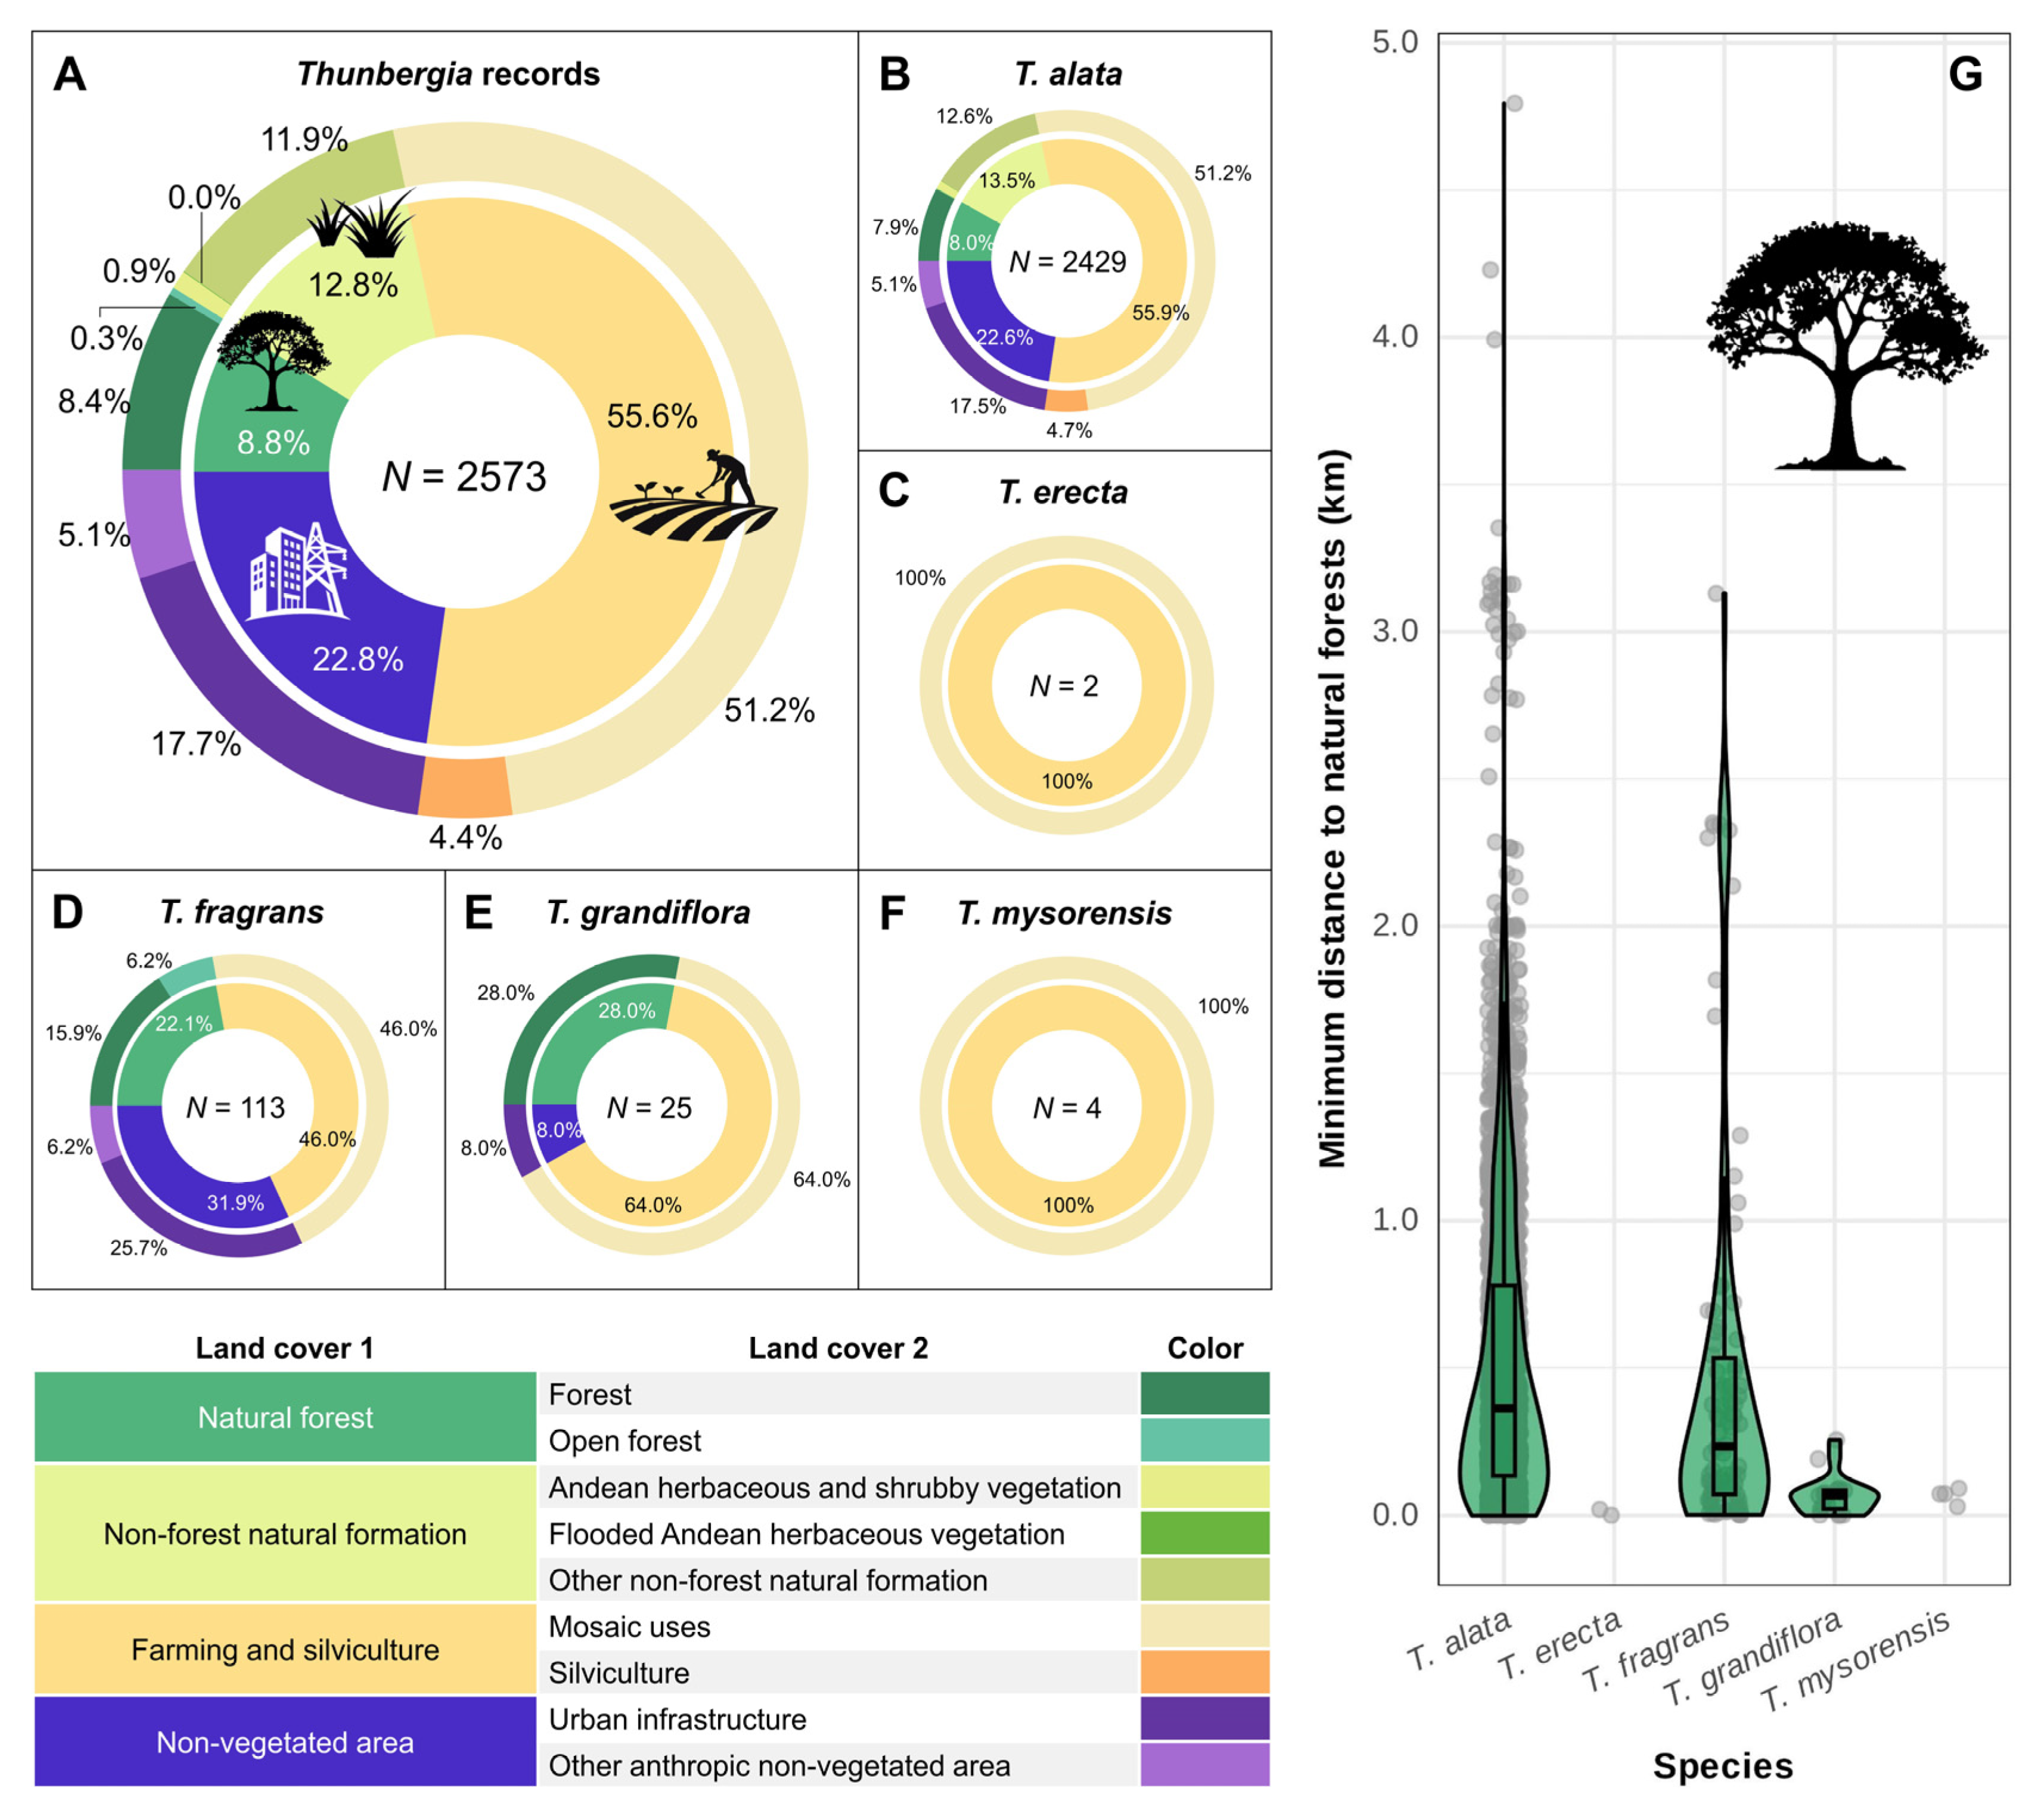
To analyze the distribution of wild Thunbergia records across different land-cover types, we overlaid the occurrences of each species (classified as casual, naturalized, invasive, or uncertain) with land-cover maps. For both continental Ecuador and the Galapagos Islands, we used data from the MapBiomas Ecuador project (3.0 collection; https://ecuador.mapbiomas.org/mapas-de-cobertura-y-uso/; accessed on 9 May 2025), which provides 40 annual land-cover layers corresponding to the years 1985–2024. MapBiomas Ecuador classifies land cover using a hierarchical system with two levels: general categories (Land cover 1) and specific classes within each category (Land cover 2). The land-cover categories and classes considered were as follows: (1) Natural forests (forests, open forests, mangroves, and flooded forests); (2) Non-forest natural formations (non-forest natural flooded formations, grasslands, Andean herbaceous and shrubby vegetation, flooded Andean herbaceous vegetation, rocky outcrops, and other non-forest natural formations); (3) Farming and silviculture (mosaic uses [croplands/pastures], silviculture, and banana plantations); (4) Non-vegetated areas (urban infrastructure, mining areas, beaches, dunes and other sandy areas, other anthropic non-vegetated areas, and other natural non-vegetated areas); (5) Water bodies (rivers, lakes and oceans, glaciers, and aquaculture areas). Because both land cover and species records vary over time, each occurrence was evaluated against the map corresponding to its year of observation. Occurrences falling within the water body category from MapBiomas Ecuador were reassigned to the nearest terrestrial land-cover type to better reflect the actual habitat context. Additionally, a proximity analysis was conducted to assess the spatial relationship between the records located outside natural forests and forested areas. Using QGIS version 3.38.3, we calculated the minimum distance from each non-forest occurrence to the nearest polygon classified as natural forest based on the 2024 MapBiomas Ecuador layer.
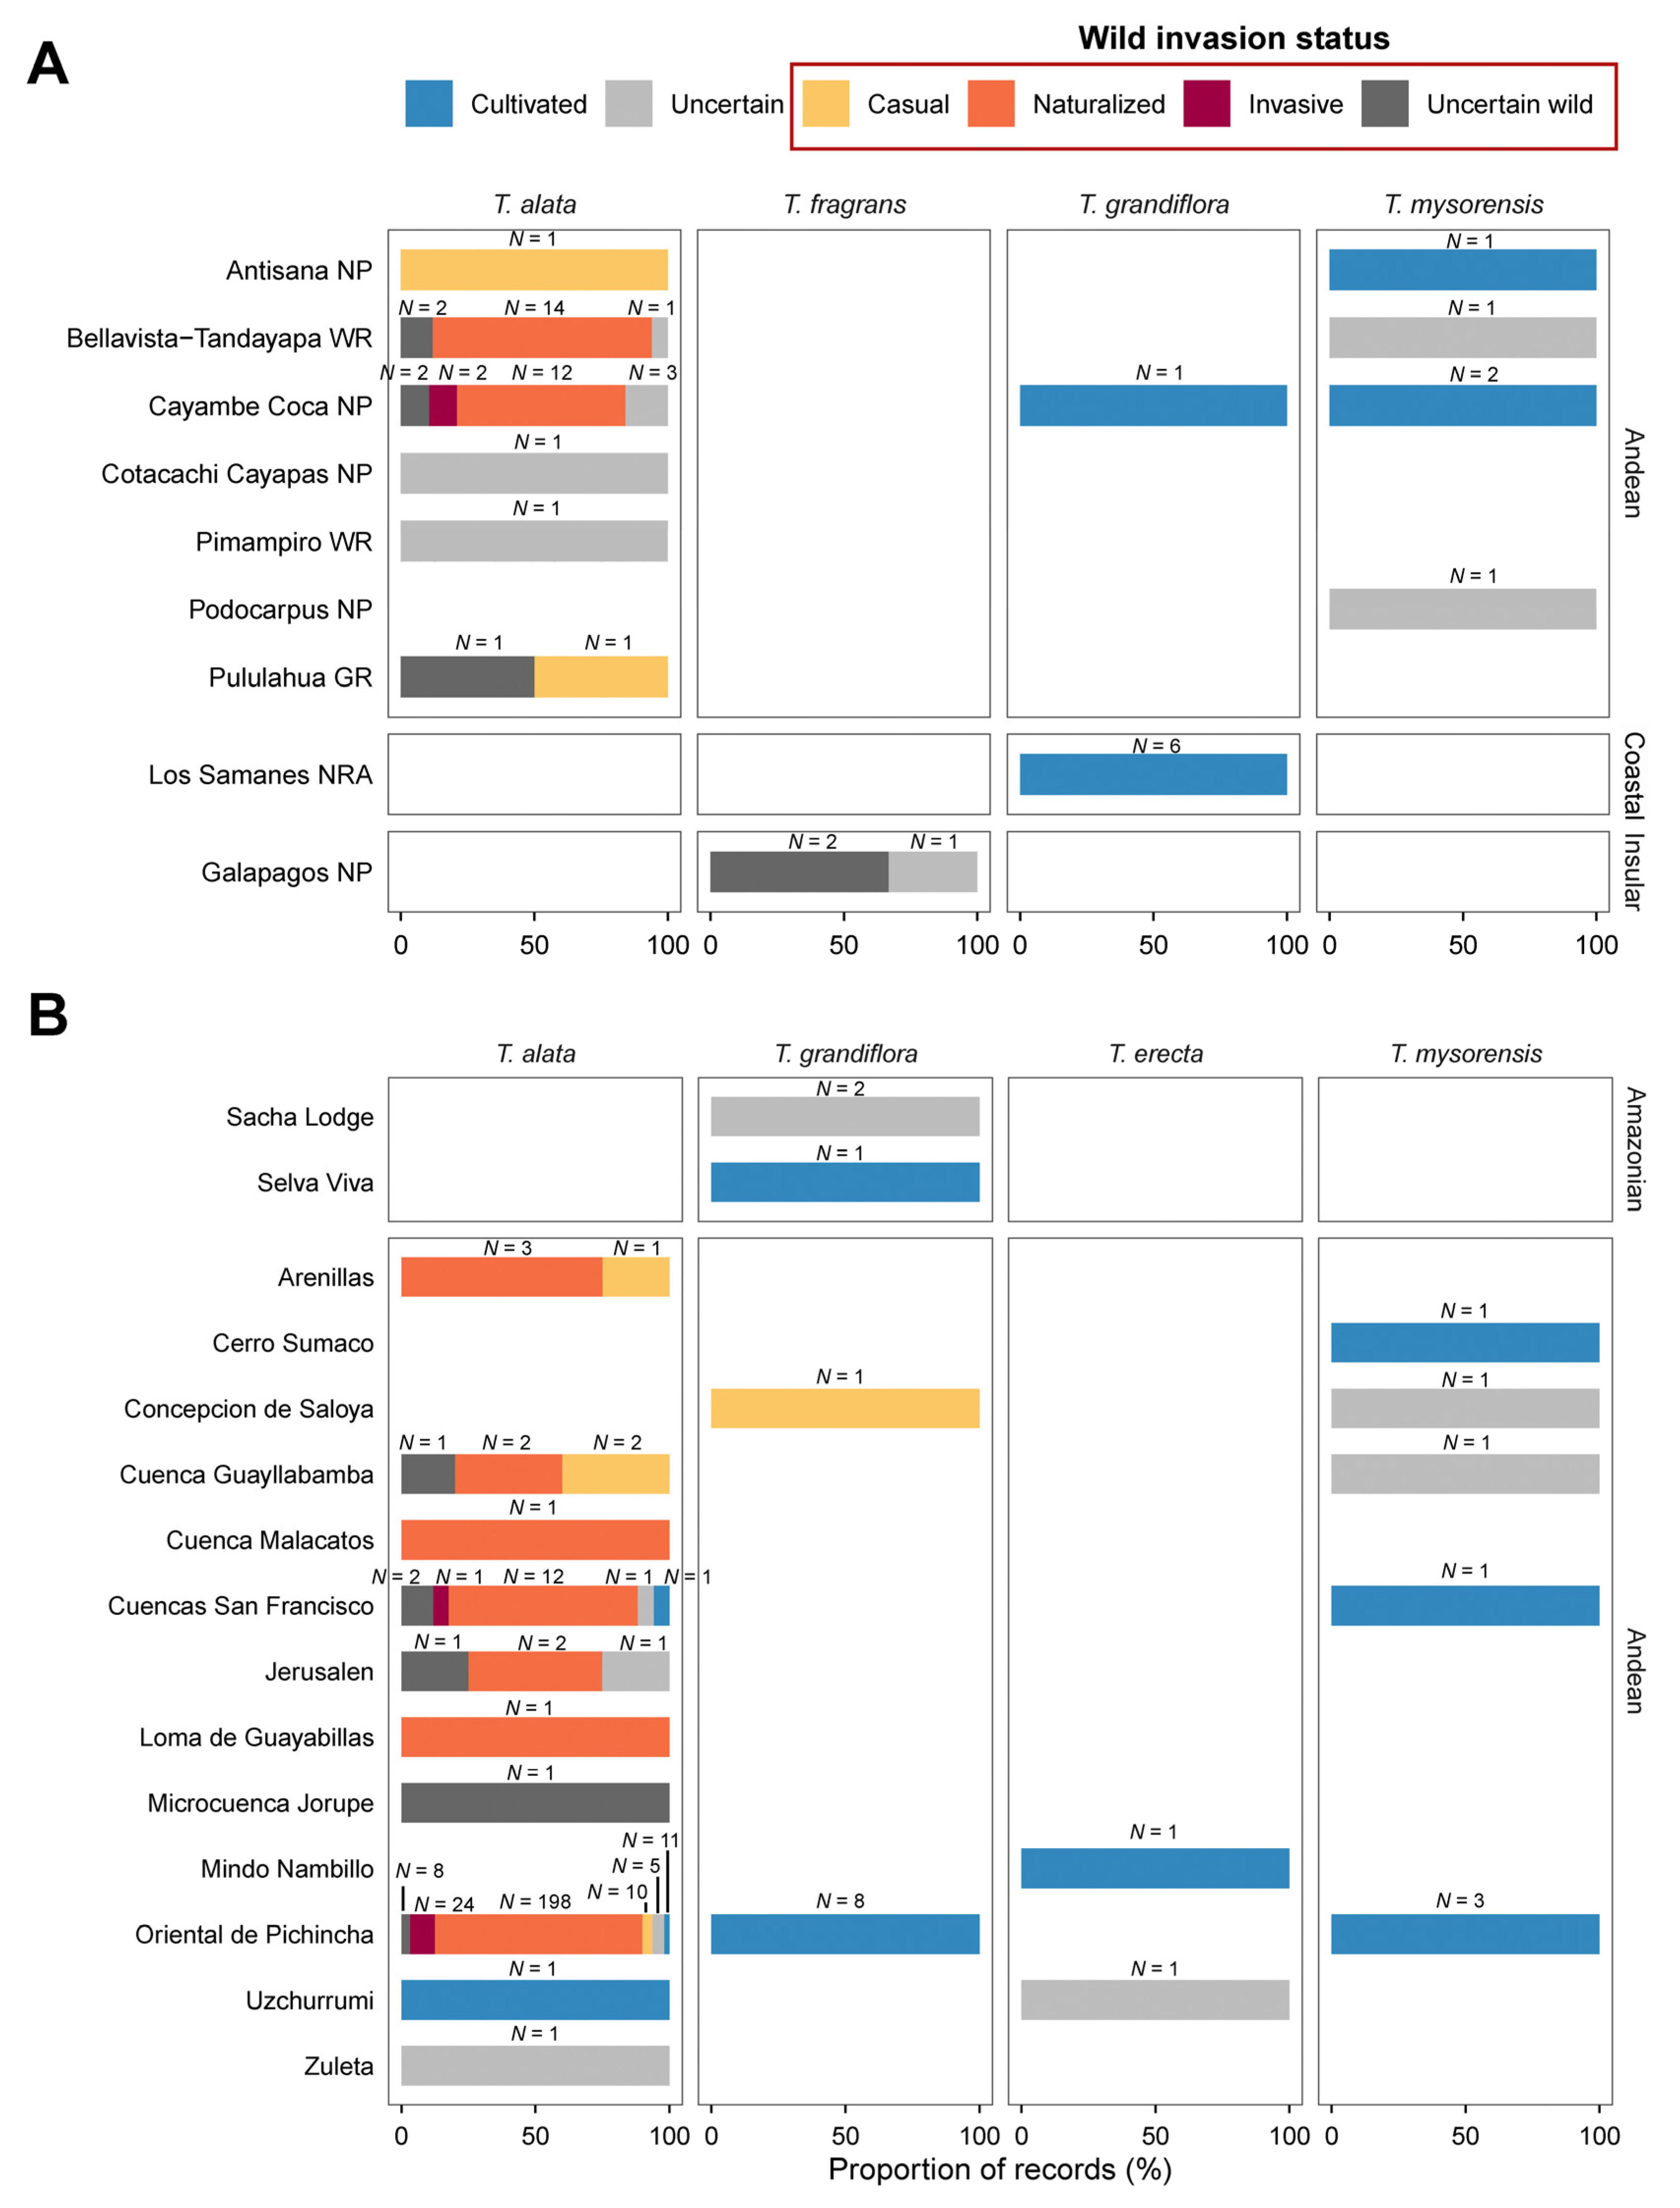
The presence and invasion status of Thunbergia species within conservation areas were assessed by intersecting georeferenced occurrence records of high spatial precision with the SNAPs and ABVP layers from the official MAATE repository [39]. Confirmed records were classified as cultivated, wild, or uncertain, with wild records further subdivided into casual, naturalized, invasive, or uncertain. This procedure enabled the identification of conservation areas where Thunbergia species are present and the characterization of their invasion status.

3. Results

3.1. General Description of the Dataset

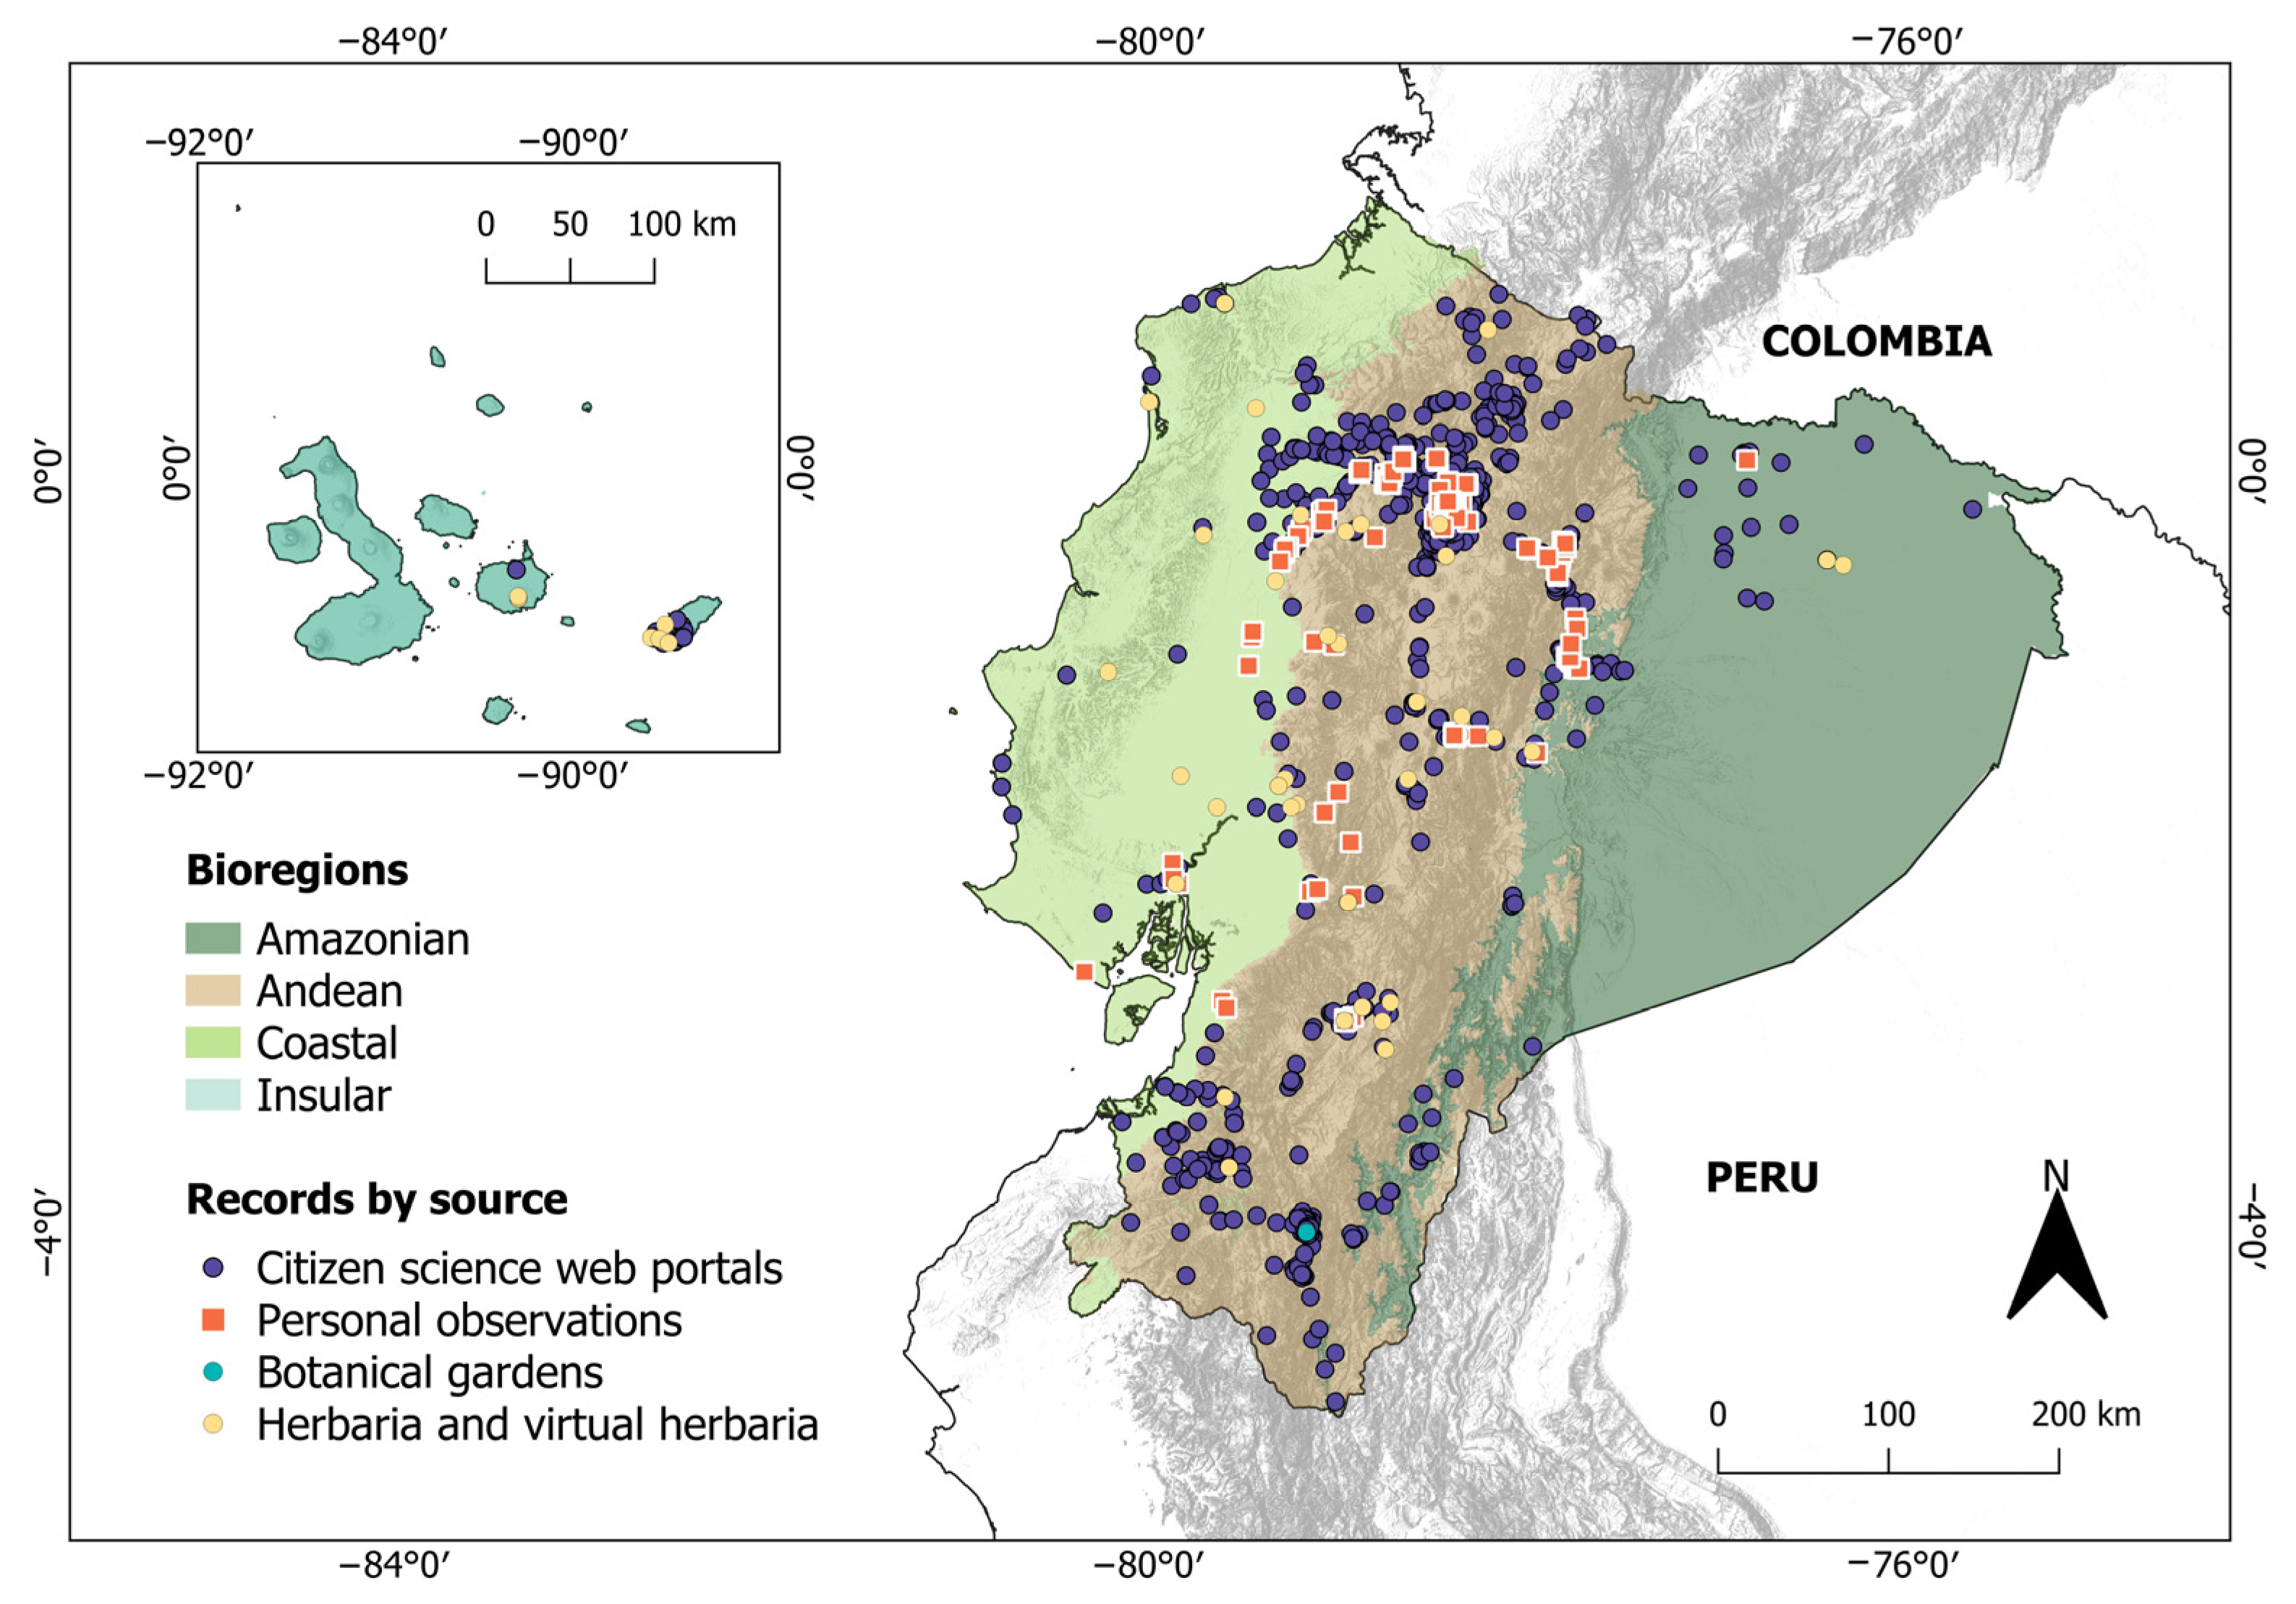
A total of 3937 verified records of Thunbergia were compiled for Ecuador (Supplementary Materials, Table S1). Of this total, 89.8% corresponded to citizen science observations (99.6% from iNaturalist), 8.6% to personal field observations, 1.5% to preserved specimens from national and international herbaria, and 0.05% to living specimens in botanical gardens (Figure 1). Additionally, 20.8% of the records from citizen science were verified in the field. Species-level identifications or taxonomic corrections were made for 88 iNaturalist records and 11 herbarium specimens.

3.2. Checklist of Thunbergia Species

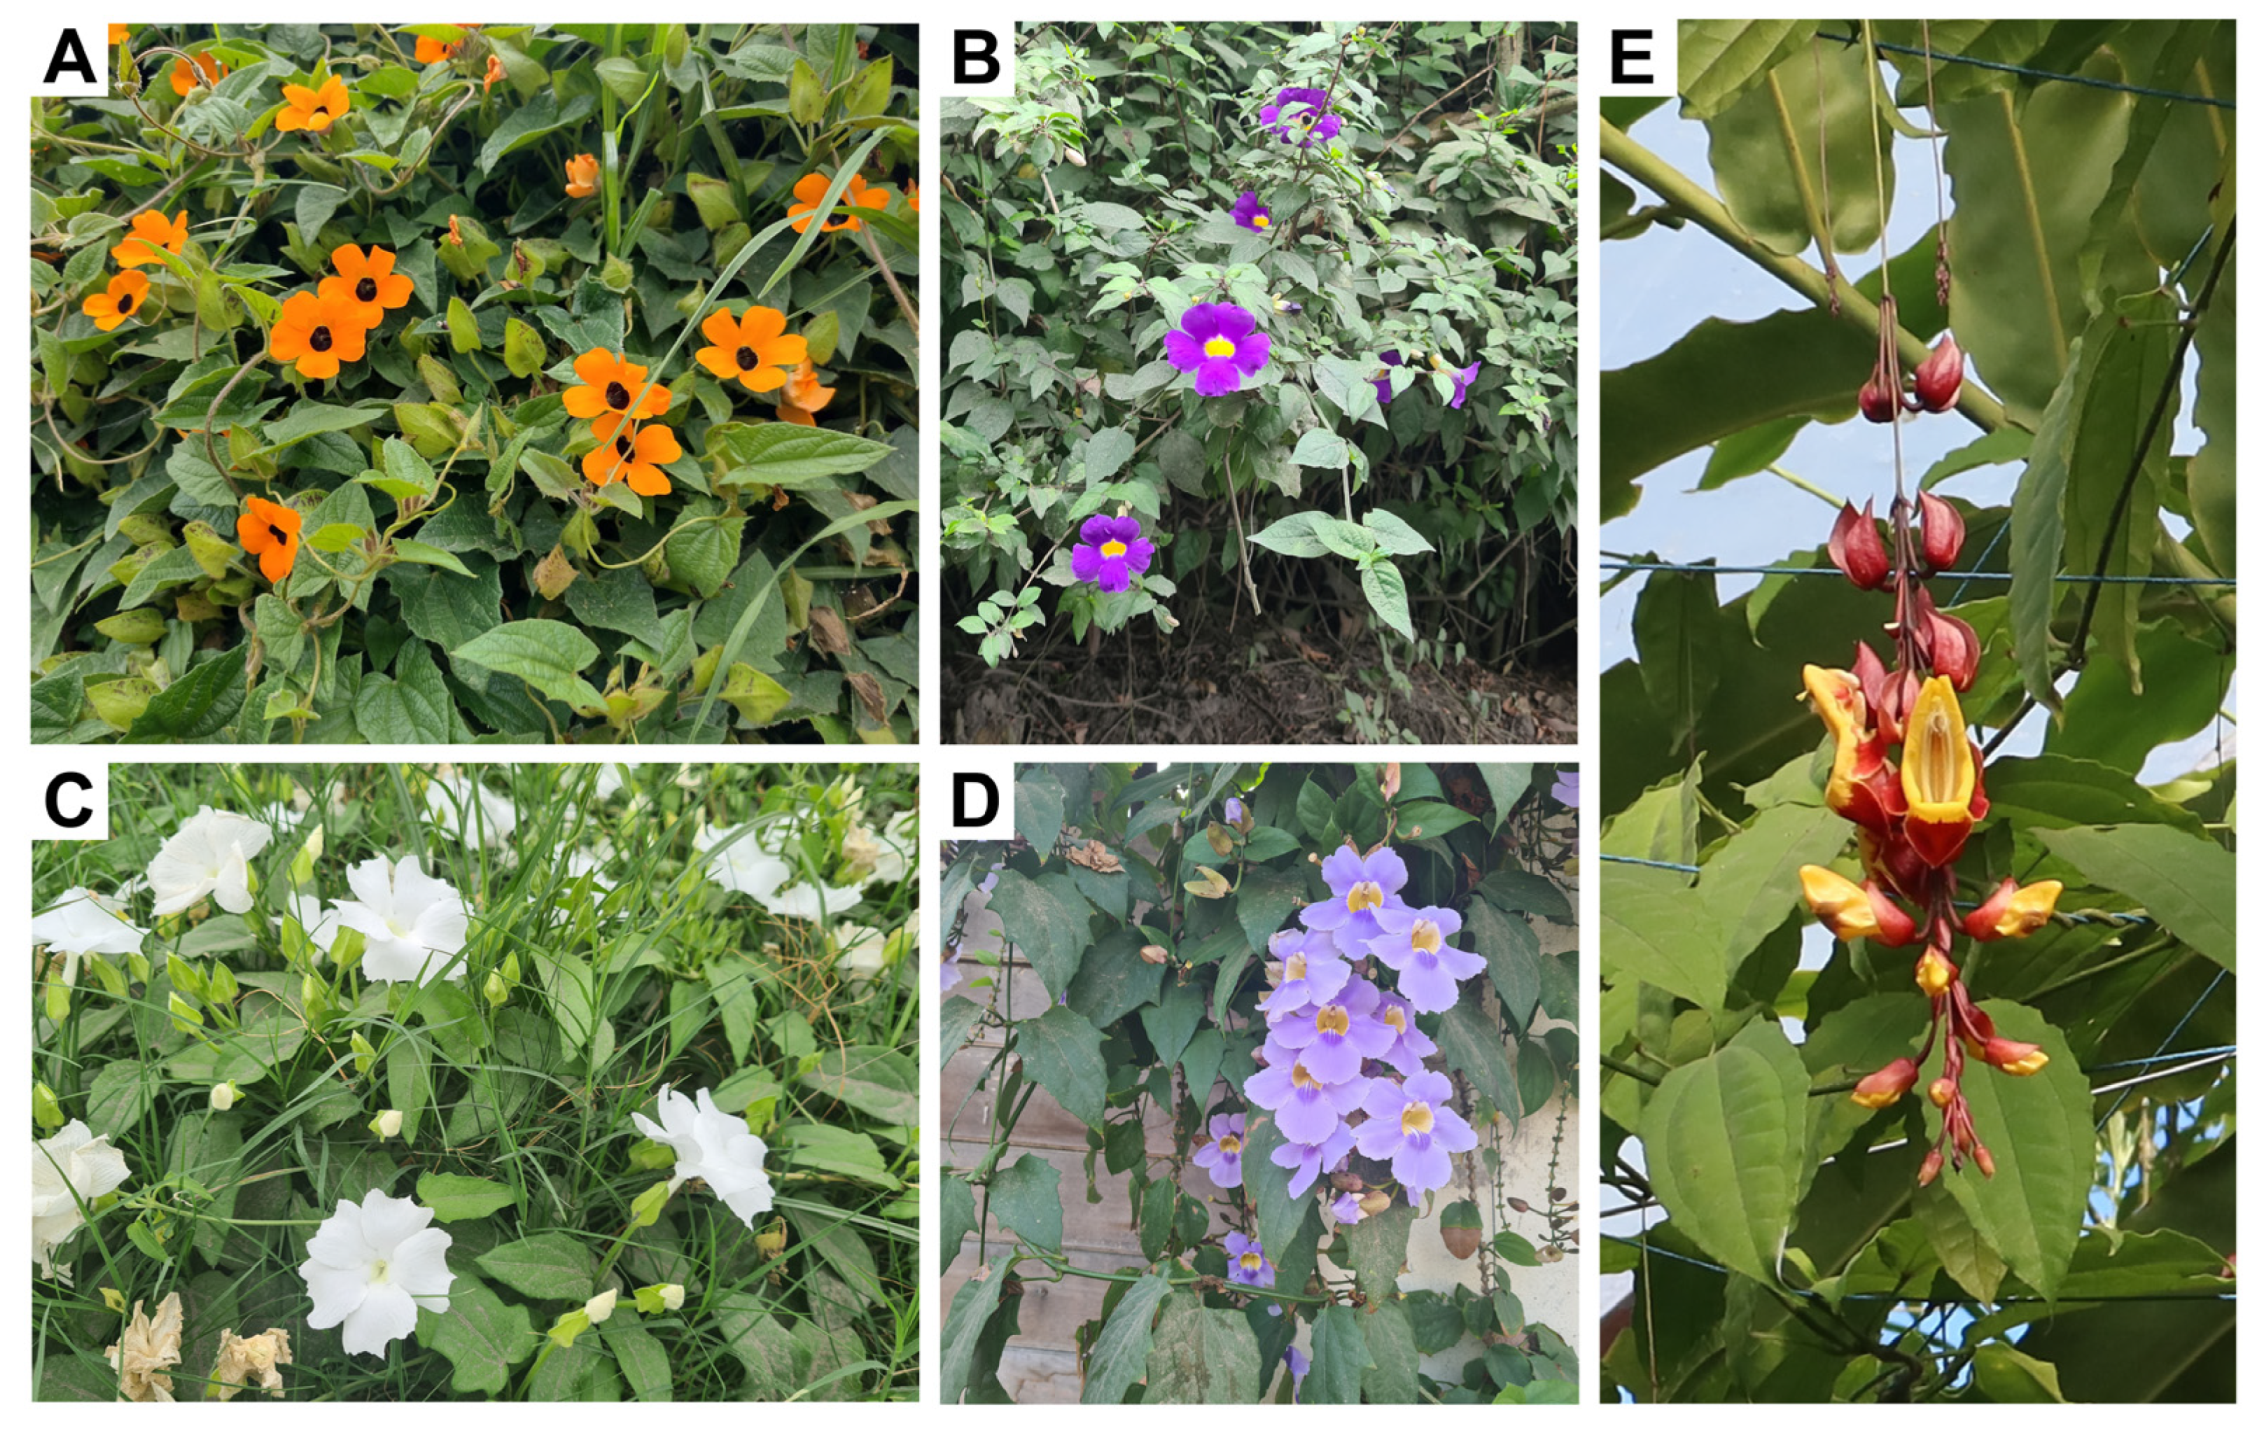
The presence of five species of Thunbergia was confirmed in the country: T. alata, T. erecta, T. fragrans, T. grandiflora, and T. mysorensis (Figure 2). The diagnostic morphological features distinguishing the five species are summarized in the following taxonomic key:
1a. Erect shrub.T. erecta
1b. Climbing or twining vines.2
2a. Petiole narrowly winged. Flowers orange or yellow, rarely white or pink, often with a black (rarely white) eye-like throat.T. alata
2b. Petiole not winged. Corolla blue, scarlet, white, or yellow.3
3a. Flowers solitary. Corolla white.T. fragrans
3b. Flowers solitary (T. grandiflora) or in terminal or axillary racemes (T. grandiflora, T. mysorensis); corolla other than white.4
4a. Trumpet-shaped flowers, corolla bluish-lilac, throat yellowish or whitish.T. grandiflora
4b. Elongated, tubular flowers, corolla lobes scarlet, tube and throat bright yellow.T. mysorensis

3.3. Spatio-Temporal Distribution of Records

Thunbergia alata represented 77.1% of the total records, followed by T. mysorensis (8.7%), and T. fragrans (5.8%) (Table 1). Most records (98.3%) were from continental Ecuador, with only 1.7% from the Insular bioregion (Galapagos Islands). For continental Ecuador, all five species were present in the three bioregions; within these, the Andean bioregion concentrated 89.4% of all Ecuadorian records, while the Amazonian and Coastal bioregions accounted for 4.6% and 4.2%, respectively. In the Galapagos Islands, only two species (T. fragrans and T. erecta) were recorded (Table 1).
Thunbergia alata had the highest proportion of records in the Andean bioregion (76%; N = 2990), with far fewer records for the Coastal (N = 25) and Amazonian (N = 18) bioregions. A similar pattern of predominance in the Andes, with lower representation in the Coastal and Amazonian, was observed for both T. mysorensis and T. grandiflora. Thunbergia erecta was more evenly distributed across the continental bioregions, with fewer records in the Insular bioregion (N = 4). Thunbergia fragrans was the only species recorded broadly across all four bioregions, showing a more balanced distribution: Andean (N = 74), Insular (N = 63), Coastal (N = 42), and Amazonian (N = 47) (Table 1).
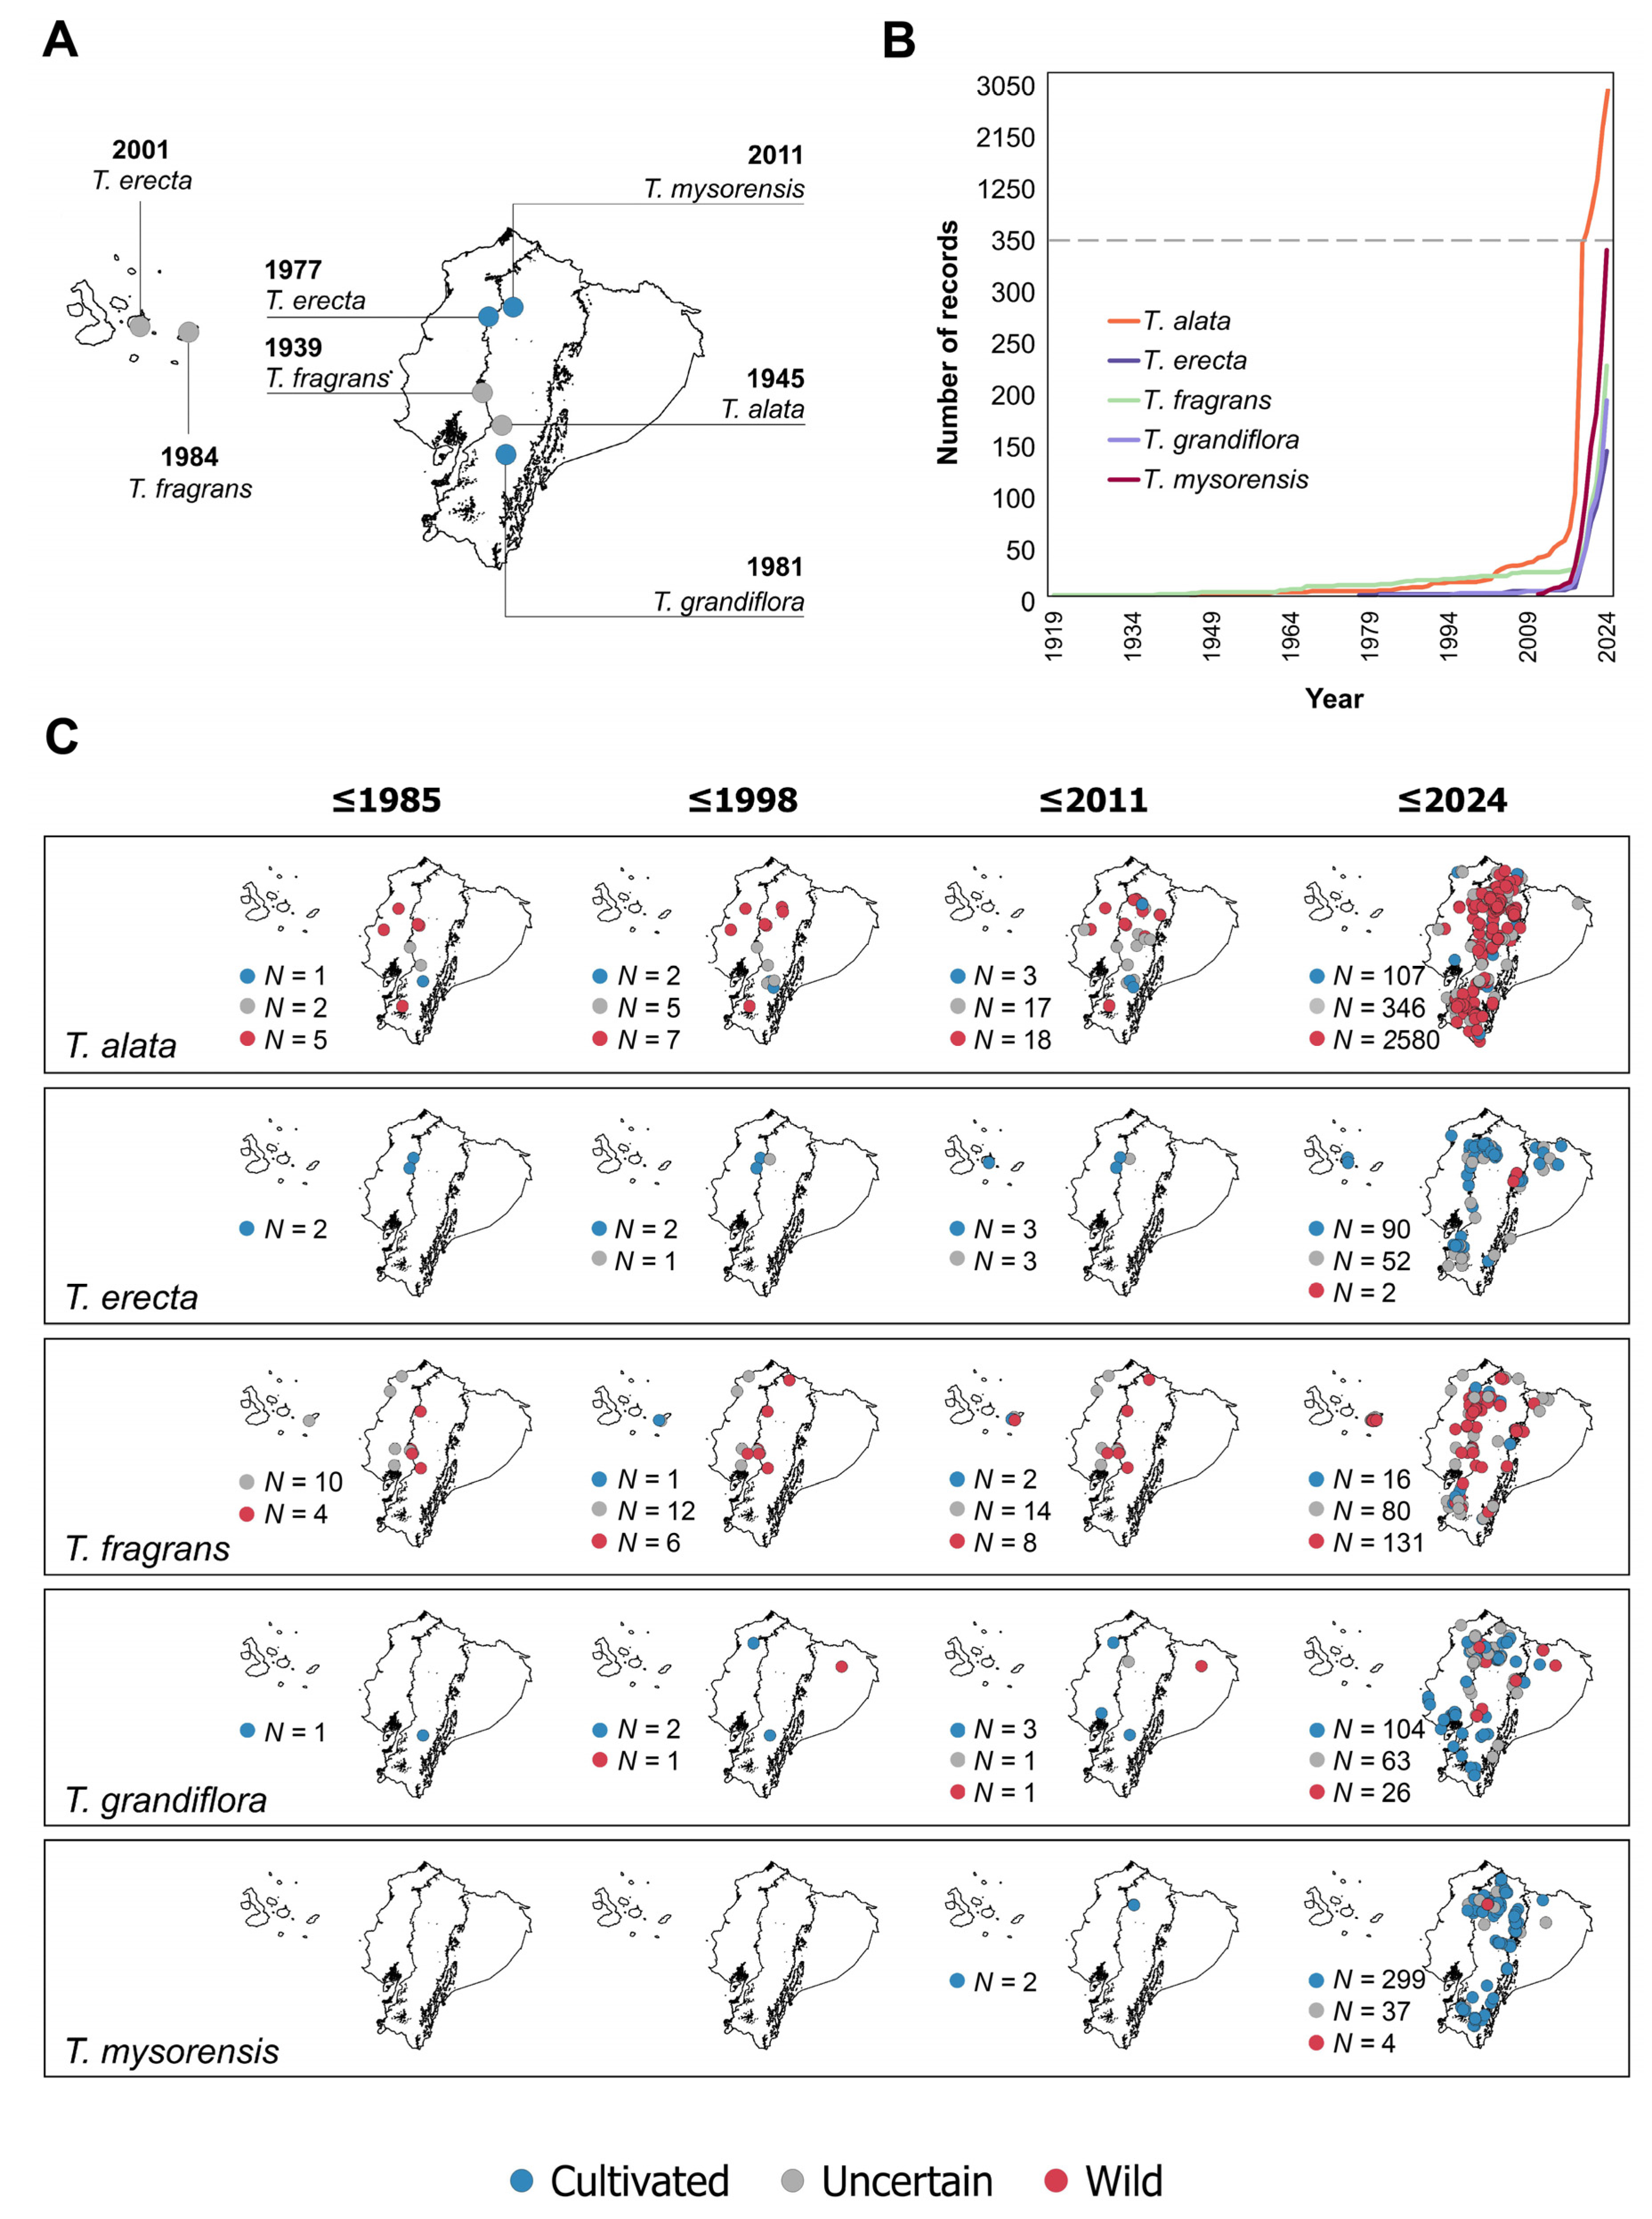
In both continental Ecuador and the Galapagos Islands, the earliest records for all Thunbergia species were classified as either cultivated or of uncertain status (Figure 3A). The earliest record of the genus in Ecuador corresponds to a specimen of T. fragrans collected in 1919 (status and location uncertain) and preserved at the United States National Herbarium (Museum of Natural History, Smithsonian Institution) (Figure 3A; https://www.gbif.org/es/occurrence/1852132849; accessed on 2 May 2024). The second-oldest record of T. fragrans, dated 1939, also has an uncertain status but a known location and is likewise preserved at the same institution (Figure 3A; https://www.gbif.org/es/occurrence/1852129245; accessed on 2 May 2024). The oldest record of T. alata dates back to 1945 and corresponds to a specimen with uncertain status preserved at the New York Botanical Garden Herbarium (Figure 3A; https://www.gbif.org/es/occurrence/1927885672; accessed on 2 May 2024). The first record of T. erecta is from 1977, represented by a cultivated specimen at the Missouri Botanical Garden Herbarium (Figure 3A; https://www.gbif.org/es/occurrence/1260463293; accessed on 2 May 2024). For T. grandiflora, the oldest recorded specimen is a cultivated plant from 1981, also preserved at the Missouri Botanical Garden Herbarium (Figure 3A; https://www.gbif.org/es/occurrence/1260382172; accessed on 2 May 2024). No herbarium specimens of T. mysorensis were found; its earliest record corresponds to a cultivated observation uploaded to iNaturalist in 2011, making it the most recently documented species of the genus in Ecuador (Figure 3A; https://www.inaturalist.org/observations/21202417; accessed on 9 January 2025).
Of the two species that were detected in the Galapagos Islands, the first documented records correspond to T. fragrans from 1984 and T. erecta from 2001 (Figure 3A), respectively. Both records are based on specimens deposited in the Herbarium of the Charles Darwin Foundation (T. fragrans: https://datazone.darwinfoundation.org/images/checklist/CDS_4279B.jpg, accessed on 3 February 2026; T. erecta: https://datazone.darwinfoundation.org/images/checklist/CDS_17964A.jpg, accessed on 3 February 2026).
The number and geographic range of Thunbergia records in Ecuador increased markedly over time (Figure 3B,C). Prior to 1985, records were scarce and restricted to the Andes and the Coast (Figure 3C). Except for T. mysorensis, gradual increases were observed between 1985 and 2011, followed by a pronounced expansion from 2011 to 2024 (Figure 3B). During this latter period, records encompassed the three continental bioregions (Amazonian, Andean and Coastal) and two species were documented in the Galapagos Islands (Figure 3C). Thunbergia alata exhibited the earliest and most pronounced expansion and is currently widely distributed across continental Ecuador (Figure 3B,C). Thunbergia erecta records remained scarce until 2011, when they rose from 5 to 143 records, distributed across the Amazonian, Andean, Coastal, and Galapagos (Figure 3C). Records of T. fragrans increased mostly in the Andean and Coastal bioregions, with few additional records detected in the Amazonian and Galapagos (Figure 3C). Thunbergia grandiflora records increased from 5 to 193 records between 2011 and 2024, also distributed across all continental bioregions (Figure 3C). Thunbergia mysorensis was the most recently recorded species, increasing from 2 to 341 records since 2011, mainly cultivated in Andean and Coastal areas (Figure 3B,C).

3.4. Invasion Status

All Thunbergia species were recorded in both cultivated and wild conditions, with proportions varying by species and bioregion (Table 1). Thunbergia alata had the highest proportion of wild records (85.1%; N = 2580) across all three continental bioregions, with fewer cultivated (3.5%; N = 107) and unknown status (11.4%; N = 346) records (Table 1). Thunbergia fragrans was the only species with confirmed wild records in all continental bioregions and in Galapagos, with wild records exceeding 58% (Table 1). The remaining three species of Thunbergia showed the opposite pattern, i.e., most of their occurrences were cultivated (62.5% for T. erecta, 53.9% for Thunbergia grandiflora, and 87.9% for T. mysorensis). While there were wild occurrences in the three continental bioregions for T. grandiflora, for T. erecta and T. mysorensis, there were only wild records in the Amazon and the Andes, respectively (Table 1).
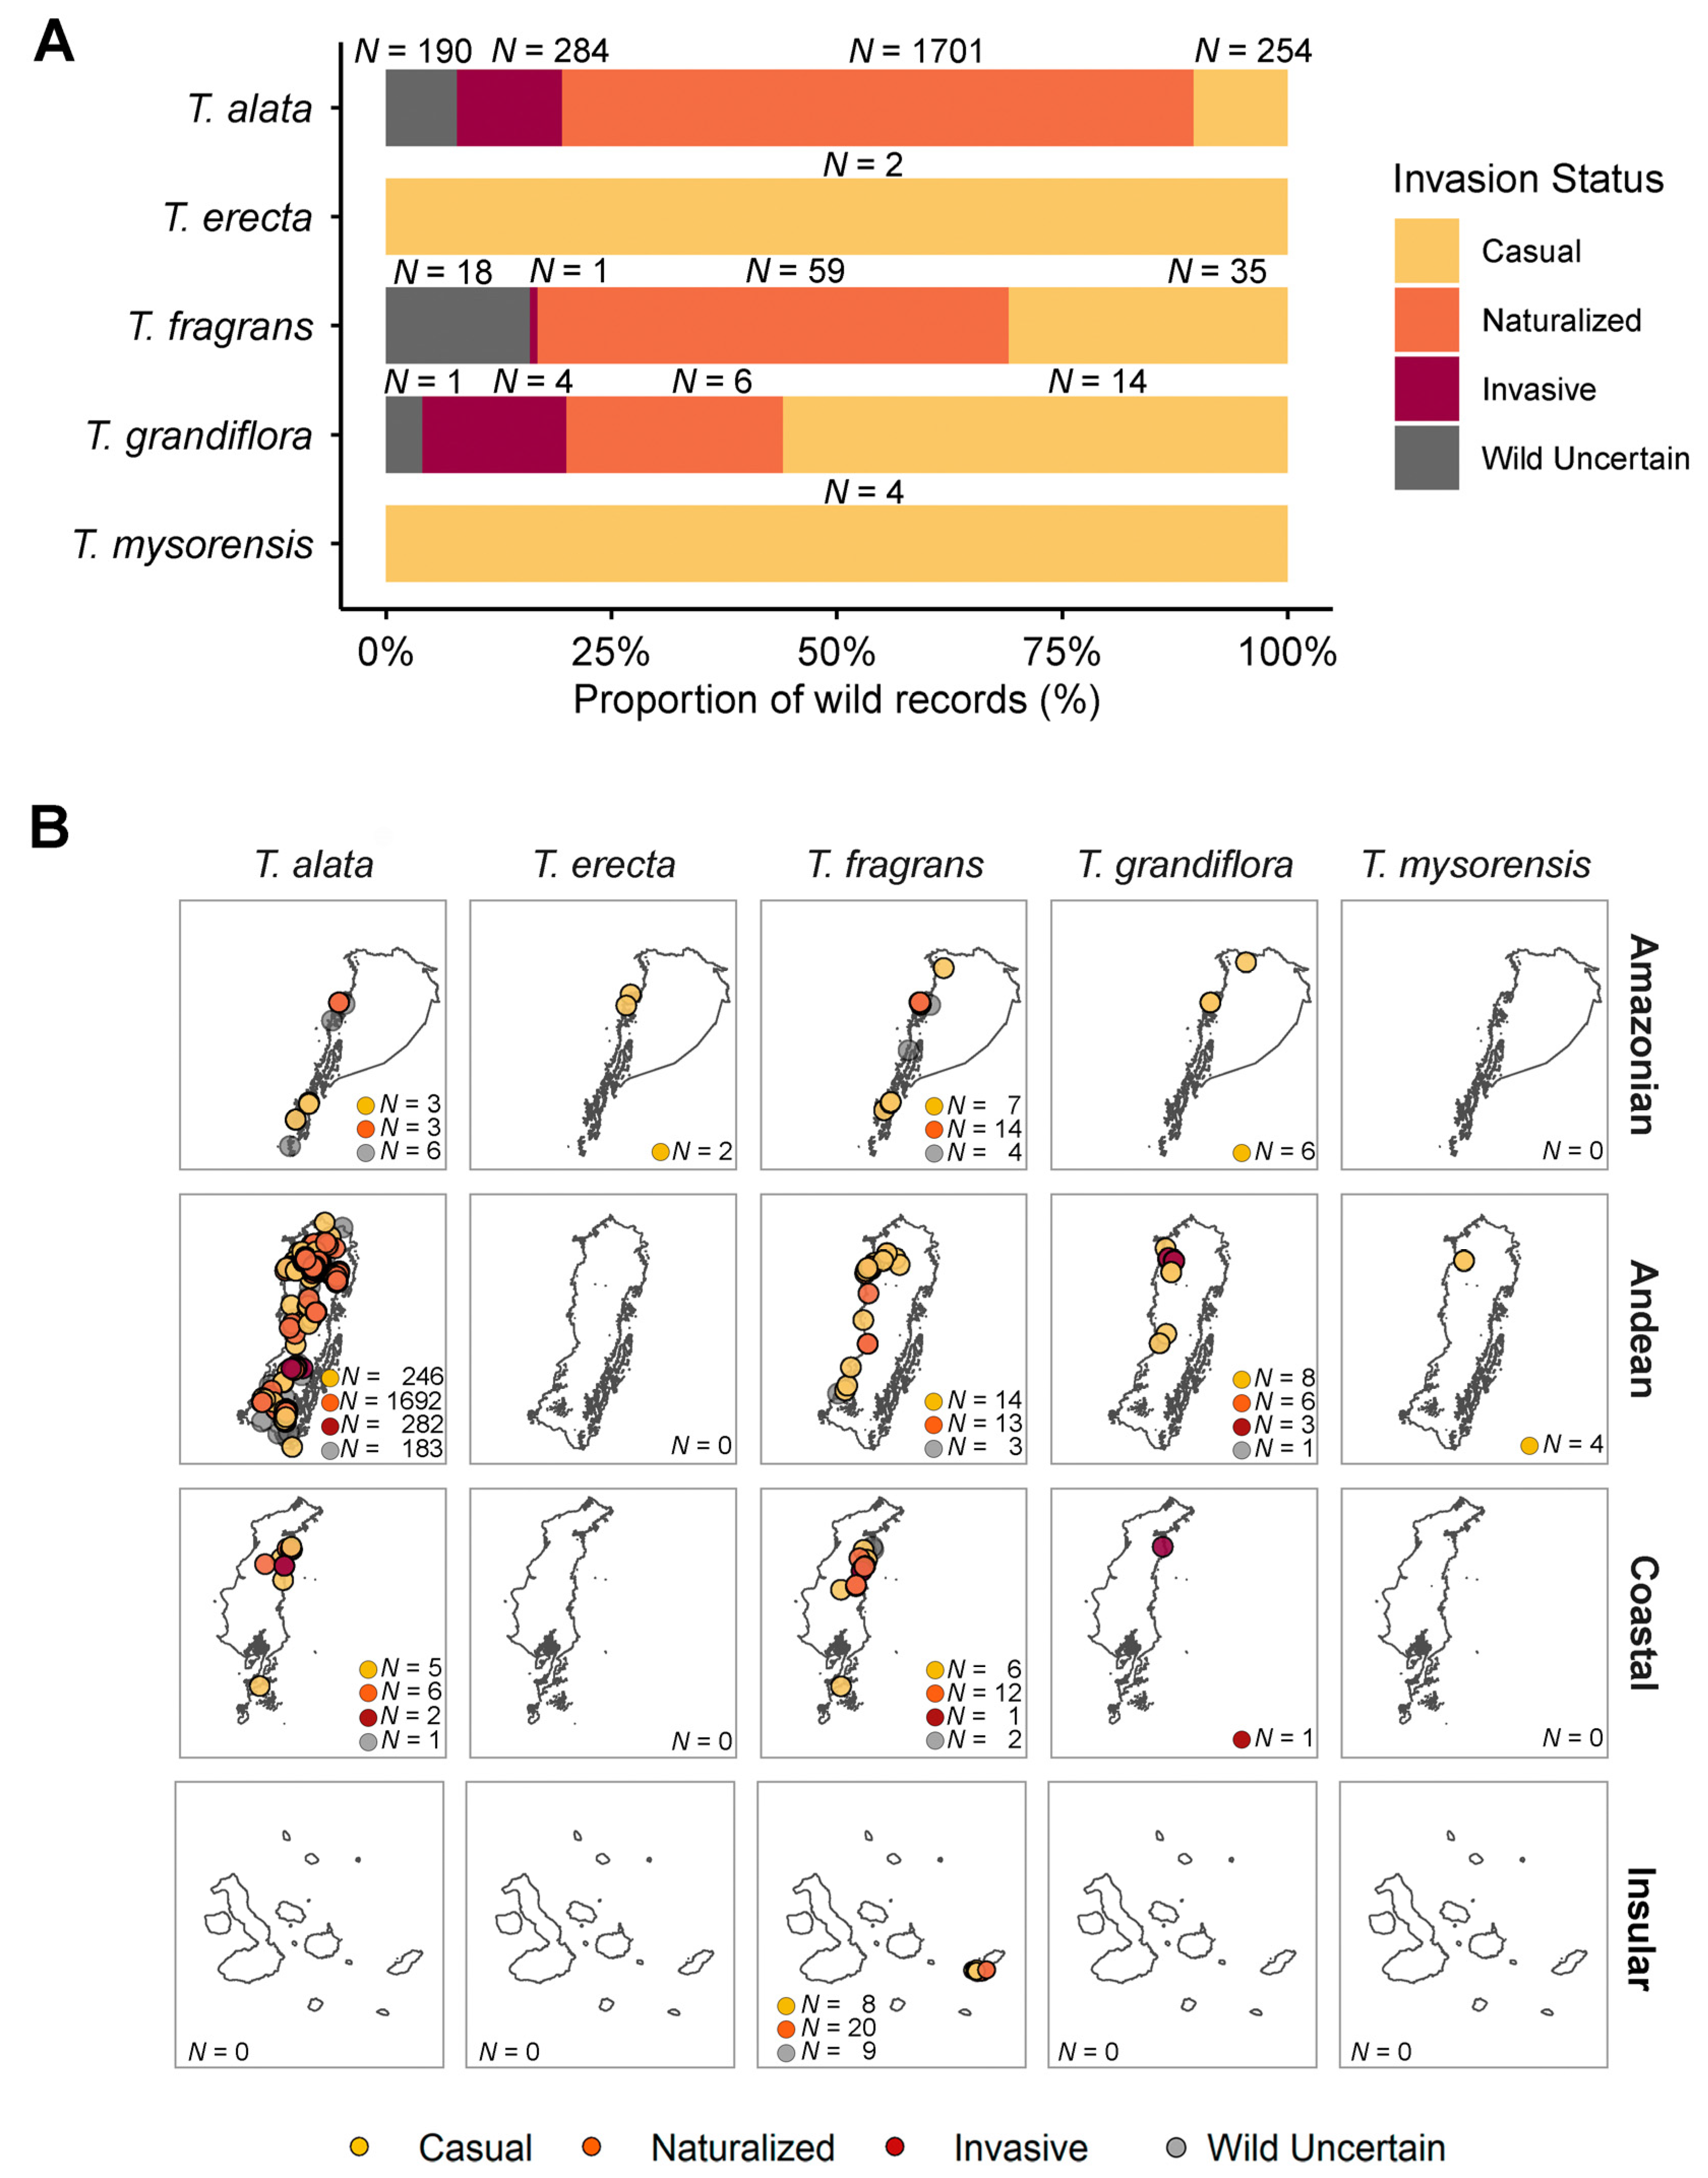
After applying the spatial precision filter (only records with precision <1 km were considered), a total of 2573 Thunbergia wild records were retained and classified according to invasion status. At the national scale, wild records revealed marked differences among Thunbergia species (Figure 4A). Thunbergia alata overwhelmingly dominated the dataset (2429 records), with most wild occurrences classified as naturalized (N = 1701; 70%), followed by invasive (N = 284; 12%), casual (N = 254; 10%), and uncertain (N = 190; 8%) (Figure 4A). In contrast, the remaining species were represented by substantially fewer wild records (2 to 113 records). Thunbergia fragrans showed the highest proportion of naturalized records (N = 59; 55%) outside T. alata, while T. erecta, T. grandiflora, and T. mysorensis had very low absolute numbers of wild records (Figure 4A).
At the bioregional scale, wild records were relatively scarce in the Amazonian bioregion (45 records), where T. alata accounted for the largest proportion, accompanied by records of T. fragrans, T. grandiflora, and the only two occurrences of T. erecta; detected for the whole country; T. mysorensis was not detected (Figure 4B). Specifically, T. grandiflora occurred exclusively as casual for the Amazonian bioregion, whereas T. fragrans and T. alata exhibited a range of invasion statuses in the wild, including naturalized, casual, and uncertain records (Figure 4B). In contrast, the Andean region showed a strong concentration of wild records (2455 records), including nearly all occurrences of T. alata—most of them naturalized and invasive—as well as a considerable part of T. fragrans records (Figure 4B). The Andes also contained scattered records of T. grandiflora and a few casual occurrences of T. mysorensis (the only four records detected for Ecuador), while T. erecta was absent (Figure 4B). In the Coastal region, only sparse records were detected (36 records), with T. alata and T. fragrans documented across several invasion status categories and a single record of T. grandiflora; no wild records of T. erecta or T. mysorensis were found (Figure 4B). In the Insular bioregion (Galapagos), wild records were restricted exclusively to T. fragrans (37 records) (Figure 4B). Overall, these patterns indicate that the Andes were the main hotspot for wild records of Thunbergia in Ecuador, while T. fragrans stood out as the only species occurring in all four regions. In summary, T. alata and T. fragrans were the dominant species in the Amazonian, Andean, and Coastal regions, whereas T. fragrans was the only species recorded in the Galapagos. Thunbergia grandiflora, T. erecta, and T. mysorensis were represented by very few wild records overall, remaining restricted to scattered or early-stage occurrences.

3.5. Environmental Preferences

A total of 2406 records of Thunbergia with a spatial uncertainty of less than 1 km occurrences were analyzed in relation to nine selected bioclimatic variables. The majority of records corresponded to T. alata (N = 2262), followed by T. fragrans (N = 113), T. grandiflora (N = 25), T. mysorensis (N = 4), and T. erecta (N = 2). Due to their limited number of records T. mysorensis and T. erecta were excluded from the analyses of environmental preferences.
The PCA explained 78% of the variance in the climatic dataset (Figure 5). Thunbergia alata was associated with greater diurnal and annual thermal variability (higher BIO2 and BIO7) and lower mean, maximum, and minimum temperatures (lower BIO1, BIO5, and BIO6) (Figure 5). In contrast, T. grandiflora but particularly T. fragrans clustered in warmer environments, characterized by higher BIO1, BIO5, and BIO6 and reduced thermal variability (lower values for BIO2 and BIO7; Figure 5). Regarding precipitation, T. fragrans was linked to greater seasonality (higher BIO15) than T. alata and T. grandiflora, whereas a subset of T. alata records was associated with low precipitation during the coldest quarter (BIO19), suggesting that this is not a general pattern for the species (Figure 5). Thunbergia grandiflora was the species most strongly associated with high values of BIO19, annual precipitation (BIO12) and precipitation of the wettest quarter (BIO16). The frequency histograms for these bioclimatic variables by species are available in Supplementary Materials (Figures S1 and S2).

3.6. Invasion Status Across Land-Cover Types and Conservation Areas

Overall, wild records of Thunbergia in Ecuador were primarily associated with human-modified environments. The farming and silviculture category accounted for 55.6% of the occurrences, followed by non-vegetated areas (22.8%), non-forest natural formations (12.8%), and natural forests (8.8%) (Figure 6A). Records of T. alata (N = 2429) were mainly concentrated in mosaic uses (51.2%), urban infrastructure (17.5%), and other non-forest natural formations (12.6%) (Figure 6B). Smaller proportions were found in forests (7.9%), silviculture (4.7%), Andean herbaceous and shrubby vegetation (0.9%), and open forests (0.1%), with a single record in the flooded Andean herbaceous vegetation (Figure 6B). Thus, Thunbergia alata exhibited the widest environmental range of land cover among Thunbergia species, as it was the only one being present across all nine land-cover subcategories considered (Figure 6B). Wild occurrences of T. fragrans (N = 113) were predominantly associated with mosaic uses (46.0%), urban infrastructure (25.7%), and forests (15.9%), with minor representation in open forests (6.2%) and other anthropic non-vegetated areas (6.2%) (Figure 6D). For T. grandiflora (N = 25), most records were also found in mosaic uses (64.0%), followed by natural forests (28.0%) and urban infrastructure (8.0%) (Figure 6E). Finally, wild records of T. mysorensis (N = 4) and T. erecta (N = 2) were restricted to landscapes with mosaic uses (Figure 6C,F). When considering only the records located outside the natural forest category, the minimum distance to the nearest natural forest varied among species (Figure 6G). The median distance was 0.36 km for T. alata, 0.26 km for T. fragrans, and 0.07 km for T. grandiflora.
All five Thunbergia species were recorded within conservation areas, although their invasion status varied among taxa (Figure 7). In the Andean region, T. alata was the most widespread species, documented in six protected areas (Figure 7A) and ten protected forests (Figure 7B). It was classified as invasive in Cayambe Coca National Park, Cuencas de los Ríos San Francisco, San Ramón y Sabanilla, Flanco Oriental de Pichincha, and Cinturón Verde de Quito, and as naturalized, casual, uncertain, or cultivated in several other Andean conservation units (Figure 7B). For T. fragrans, three records classified as uncertain or uncertain in the wild were confirmed in Galapagos National Park (Figure 7A). A few records of T. erecta were reported as cultivated or uncertain in two protected forests (Figure 7B). We also confirmed the presence of T. grandiflora in two protected areas, both classified as cultivated (Figure 7A). This species additionally appeared as cultivated or of uncertain status in three protected forests, with a single naturalized record in the protected forest Concepción de Saloya (Figure 7B). Finally, T. mysorensis was recorded in four protected areas and five protected forests, with no confirmed wild occurrences; all records were categorized as cultivated or of unknown status (Figure 7A,B).

4. Discussion

This study provides the first nationwide assessment of Thunbergia species in Ecuador. Five species were confirmed in continental Ecuador (T. alata, T. erecta, T. fragrans, T. grandiflora, and T. mysorensis), two of which (T. erecta and T. fragrans) also occur in the Galapagos Islands. All species were recorded both in cultivation and in the wild, indicating that the ornamental trade represents the primary pathway for the introduction and spread of this genus in Ecuador. Three species, T. alata, T. fragrans, and T. grandiflora, were categorized as invasive in Ecuador. Most records originated from citizen science platforms, primarily iNaturalist, highlighting the growing value of public participation in documenting under-sampled and fast-spreading taxa. Most of the wild records (>75%) corresponded to T. alata, showing clear evidence of naturalization and invasion in Andean regions, including protected areas. Although often associated with human-modified landscapes, its presence in native forests suggests that urban cultivation facilitates its establishment and spread into nearby natural habitats. Thunbergia fragrans, in turn, was the only species recorded in the wild across all bioregions, including the Galapagos, and frequently occurred in agricultural areas, where it may behave as a weed. Overall, our results illustrate a consistent invasion pathway from ornamental gardens to natural ecosystems for the genus Thunbergia and identify T. alata as an emerging threat to Andean mountain ecosystems.

4.1. Pathways of Introduction and Expansion

Invasive alien plants often share common drivers of spread, particularly strong human assistance through ornamental horticulture, which represents the primary use of non-native wild plant taxa in Ecuador [10]. Many invasive species exhibit mixed reproductive systems associated with increased invasion success [49,50]. These reproductive strategies are especially common among ornamental plants because they promote rapid growth, ease of cultivation, and prolonged flowering, traits that are also associated with increased invasion potential. Vegetative reproduction allows rapid growth and the formation of extensive monospecific patches, promoting the colonization of nearby habitats [51,52,53,54], whereas sexual reproduction enhances long-distance dispersal and persistence through seed banks [51,55]. In addition, horticultural selection of ornamental genotypes with fast vegetative growth or prolonged flowering may further increase their spread potential [56,57]. All five recorded species of Thunbergia are cultivated for ornamental purposes. Among them, T. alata, T. erecta, T. grandiflora, and T. mysorensis are widely commercialized in nurseries, while T. grandiflora and T. mysorensis and are frequently planted at high density in butterfly houses, birdwatching centers, botanical gardens, and private ecological reserves to attract wildlife and enhance landscape esthetics (A. Reyes-Hernández, pers. observ.). This intensive cultivation explains the concentration of records in urban, peri-urban, and other human-modified environments, whereas favorable reproductive traits facilitate the escape of cultivated individuals into natural and semi-natural ecosystems, identifying ornamental horticulture as the main introduction pathway for the genus Thunbergia in Ecuador.
Another important escape pathway involves the disposal of vegetative material in pruning waste, particularly along roadsides, ravines, and peri-urban areas, which promotes vegetative propagation and facilitates the escape of Thunbergia from cultivation [25,58,59]. Waste-disposal sites are widely recognized as sources of exotic plant propagules capable of spreading into adjacent natural habitats [60,61]. This mechanism is particularly relevant for T. erecta, T. grandiflora, and T. mysorensis, which have not been observed fruiting in Ecuador (A. Reyes-Hernández, pers. observ.). Furthermore, field experiments conducted in Guangzhou (southern China), where T. grandiflora was introduced, reported a fruit set of 0% under artificial cross-pollination, self-pollination, and natural pollination treatments [62]. These results suggest that the spread of T. grandiflora, categorized as invasive in this study, relies primarily on vegetative reproduction and human-mediated dispersal of plant fragments [62,63]. Indeed, modifications to reproductive systems are not rare during plant invasions, with several documented cases of species that become entirely or functionally asexual outside their native ranges (generally due to founder effects or the absence of compatible mates or pollinators), e.g., Arundo donax [64] or Oxalis pes-caprae [65]. The ornamental use of T. grandiflora thus drives both its introduction and spread, while improper management of pruning waste further promotes its expansion and should be considered in management strategies. In contrast, T. alata and T. fragrans combine sexual and asexual reproductive strategies with long-distance seed dispersal, which together facilitate their expansion. Both species were frequently observed fruiting in the field (A. Reyes-Hernández, pers. observ.), although studies assessing seed viability and germination rates at the local scale are still lacking. Likewise, both species propagate asexually through stem and root fragments [58,59]. In the Central Andes of Colombia, T. alata shows high germination percentages, short germination times, and seeds with prolonged viability, suggesting the formation of persistent seed banks [66]. Although improper management of pruning waste may also contribute to the spread of these species, their capacity for sexual reproduction combined with long-distance seed dispersal is likely to increase propagule pressure, making the management of these two invasive species more complex.
The first casual wild records of T. erecta and T. mysorensis in Ecuador originated from field observations of previously cultivated individuals abandoned for more than ten years. Thunbergia mysorensis was found escaping cultivation and climbing trees up to 11 m tall. iNaturalist users, as well as local residents and staff from tourist reserves, particularly in Mindo (Pichincha, near Quito), reported seeing this species growing wild on several occasions and often believed it to be native, frequently confusing it with an orchid. Thunbergia mysorensis has only been reported as subspontaneous on Réunion Island [20], in New Caledonia [67], in Australia [68], in Guatemala [69], and in Guadeloupe of the Lesser Antilles [70], with no other records as a non-native wild species to our knowledge; therefore, its casual records in Ecuador may represent an early stage of establishment and warrant further monitoring and assessment of its invasive potential.

4.2. The Role of Citizen Science in Documenting Thunbergia Invasions

Citizen science played a key role in this study, providing most of the data used to assess the distribution and invasion status of Thunbergia species in Ecuador. Approximately 90% of all records were obtained from the iNaturalist platform, greatly exceeding the coverage provided by herbarium specimens or traditional field surveys. The marked increase in Thunbergia records after 2019 coincides with the launch of the iNaturalistEC initiative by the National Institute of Biodiversity (INABIO), which substantially increased public participation in documenting the national flora. This strong reliance on citizen-generated data highlights the growing importance of participatory monitoring for documenting poorly sampled taxa and rapidly spreading ornamental invaders [43,71,72,73]. Citizen science also facilitated the detection of Thunbergia species not previously included in national checklists, revealing gaps in existing inventories. For T. mysorensis, nearly all records, including the first record for the country, were obtained from iNaturalist; the only additional record corresponds to a living specimen in a botanical garden, and no herbarium specimens are currently available for this species.
Similar patterns of effectiveness of citizen science have been reported in other studies on invasive plants. In Ecuador, the integration of iNaturalist data substantially improved updates to the lists of cultivated and wild Kalanchoe species and helped clarify their invasion status [42]. In Texas, the “Invaders of Texas” program trains volunteers to monitor invasive plants statewide, leading to the detection of previously undocumented populations of species such as Arundo donax, later validated by experts [74]. In South Africa, iNaturalist enabled the identification of 26 invasive ornamental Melaleuca species, including five species not previously recorded for the country [73]. In Spain, the iNaturalist “InvaPlant” project (https://www.inaturalist.org/projects/invaplant; accessed on 6 January 2026) has allowed recording about 40,000 occurrences of those invasive species regulated by law at both the Spanish and European Union levels in less than three years. Together, these examples show that citizen-generated data are now essential for the early detection and monitoring of invasive plant taxa.
Because iNaturalist records usually include georeferenced photographs with precise coordinates and temporal metadata, they allow verification of taxonomic identifications and support spatiotemporal analyses of invasion dynamics. These data also guided fieldwork by enabling strategic prioritization of survey efforts. Localities with high densities of cultivated individuals directed targeted surveys, which resulted in the first casual wild records of T. mysorensis and T. erecta. Likewise, iNaturalist observations were essential for locating populations of T. grandiflora and for confirming their wild status through field validation, information that would likely have remained undetected using herbarium collections alone.
The study was also strengthened by increasing public interest in the presence, escape, and spread of these species, particularly T. alata. This species received media coverage from governmental agencies (e.g., https://www.quitoinforma.gob.ec/2023/11/30/municipio-socializa-estrategias-para-erradicar-plantas-invasoras/, accessed on 3 February 2026), as well as from national and local newspapers (https://www.elcomercio.com/tendencias/ambiente/susanita-planta-invasora-bosques-quito/, accessed on 3 February 2026), radio (https://www.radiopichincha.com/susanita-la-enredadera-que-amenaza-los-bosques-y-quebradas-de-quito/, accessed on 3 February 2026), and television outlets (https://www.youtube.com/watch?v=hl2VSAa9zAg, accessed on 3 February 2026). This exposure likely motivated active participation through the provision of detailed locality data and documentation of populations at different invasion stages. Complementary observations, including repeated photographs and coordinate verification, improved the spatial resolution and accuracy of the dataset. These contributions support the idea that scientific outreach, combined with citizen science, is essential for the early detection, monitoring, and management of fast-spreading ornamental taxa such as Thunbergia. For instance, in August 2025, an eradication campaign of T. alata was carried out in the La Armenia urban park of Quito (located in the outskirts of Ilaló Volcano) thanks to the participation of up to 70 volunteer citizens (https://zonales.quito.gob.ec/?p=303875, accessed on 3 February 2026).
Despite their value, the data generated in this study show several inherent biases and limitations, most notably strong spatial clustering around populated, tourist, and easily accessible areas. Similar accessibility-driven biases have been reported in other regions, for example, in British Columbia, where more than 94% of iNaturalist observations occur within 1 km of roads [75]. These patterns are also influenced by proximity to cities, population density, land-cover type, and ecosystem zone [75,76,77,78,79]. Observations are also more frequent inside parks and protected areas than in surrounding landscapes [75]. To reduce these limitations, all records were manually curated, and a representative subset was validated through field verification. Such quality-control procedures are essential to ensure data reliability, particularly when citizen-science observations inform national assessments or management decisions. In addition to spatial biases, citizen-science records often lack information on abundance and habitat context, a limitation that is especially pronounced for ornamental species. Observers frequently photograph only conspicuous structures, such as flowers, resulting in records with limited ecological information. This limitation contributed substantially to 14.7% of the records being classified as having an uncertain status. Although spatial biases toward accessible or populated areas are inherent to most citizen science datasets, the integration of herbarium specimens, biodiversity databases, and targeted field validation contributed to improving representativeness and strengthening the robustness of the dataset.

4.3. Environmental Preferences

The results show that the three Thunbergia species evaluated largely share similar climatic conditions, with substantial overlap in their occupied environmental ranges and frequent spatial coexistence, as confirmed by field observations. Despite this shared climatic space, the analysis of climatic variables revealed consistent patterns that characterize the environments where these species are most frequently recorded. Overall, records are concentrated in climatic conditions typical of the tropical Andes, mainly associated with humid montane and piedmont environments and moderate temperatures. These conditions suggest that Andean ecosystems represent a recurrent climatic core for the establishment of Thunbergia species in Ecuador.
Thunbergia alata showed a clear concentration of records within a relatively narrow set of climatic conditions; however, compared with the other species of the genus, it was recorded across the broadest environmental gradient in the country. Most occurrences were associated with humid montane environments typical of tropical Andean forests, which concentrate the highest density of records for this species in Ecuador. The Catalog of Vascular Plants of Ecuador [80] reports its presence up to 1000 m a.s.l.; however, field observations documented naturalized populations at elevations of up to 2900 m a.s.l. in the Metropolitan District of Quito, Pichincha. This broad environmental tolerance observed in Ecuador is consistent with previous reports describing T. alata as an important invasive species under contrasting tropical and subtropical climatic conditions. Additionally, previous climate niche modeling of T. alata in Ecuador determined that the most influential bioclimatic variables are related with warm and stable temperature conditions [81]. According to Rojas-Sandoval and Acevedo-Rodríguez [26], T. alata primarily occupies tropical rainforest, monsoonal, and savanna climates, but it can also tolerate temperate conditions with minimum temperatures as low as −1 °C. In addition, the species has been reported as naturalized and invasive in humid low-elevation areas near sea level on Pacific islands [24], as well as in deciduous dry forest areas of the Andaman Islands, India, together with T. grandiflora [82]. The study of Gallagher et al. [83] demonstrated that T. alata has been able to partially shift its climate niche compared to their native areas in its invaded ranges in Australia, where it is able to grow either under cooler (temperate broadleaf and mixed forests) or drier (Mediterranean forests, woodlands and scrub) conditions. These observations underscore the importance of implementing preventive management measures in regions where the species has not yet been reported. In the case of T. fragrans, the results confirmed its naturalization across all four bioregions of Ecuador, with wild records showing a relatively homogeneous distribution, reflecting its affinity for a broad range of warm and humid climatic conditions. At a global scale, this species is mainly associated with monsoonal and savanna climates, where it tolerates both high humidity and seasonal drought, and can also persist in temperate regions with minimum temperatures close to 10 °C [84]. In Ecuador, T. fragrans is frequently reported from humid piedmont and Amazonian climates, as well as from forests in arid and semi-humid zones of the Galapagos Islands. In summary, Ecuador’s topographic and climatic diversity favors the establishment of Thunbergia species. Therefore, it is essential to consider regional climatic differences and to anticipate potential expansion beyond currently occupied areas when planning preventive management measures.
The dominance of wild Thunbergia records in human-modified landscapes highlights the central role of landscape transformation in facilitating invasion in Ecuador. Agricultural mosaics likely act as key entry points for persistence and spread, while repeated occurrences in natural forests indicate a spatial gradient of invasion extending from adjacent anthropogenic matrices [85]. This interpretation is supported by the consistently short distances of non-forest populations to forest edges, suggesting strong spatial coupling rather than independent establishment within forests. This pattern is especially relevant for T. fragrans and T. grandiflora, for which forest occurrences represent a substantial share of wild records despite low overall abundance. In contrast, T. alata exhibits broad ecological tolerance across land-cover types, consistent with its higher invasion success. Overall, this pattern provides evidence of the close linkage between anthropogenic disturbance and invasion success in ornamental taxa.
Within this landscape context, forest fragmentation emerges as a key process increasing the susceptibility of forest ecosystems to biological invasions by altering spatial configuration and expanding edge-exposed areas. The IPBES synthesis highlights that forest-edge expansion is consistently associated with higher propagule pressure and environmental conditions favoring pioneer and generalist species, many of which are non-native, potentially leading to the replacement of specialist native species [61]. This pattern has been widely documented across forest systems, where higher edge-to-interior ratios are linked to increased prevalence of invasive plants in forest fragments, regardless of forest type or region (e.g., [86,87,88]). Importantly, fragmentation does not constitute a primary introduction pathway, but rather facilitates the entry and persistence of exotic species in forested environments once they are established in the surrounding landscape [61].
Within this framework, anthropogenic infrastructure plays a central role in shaping invasion dynamics by creating linear corridors that intensify edge effects and facilitate the establishment of exotic plants along forest margins. Roads, rural tracks, and power lines are widely recognized as favorable habitats for non-native species, particularly in mountainous landscapes and protected areas [89,90,91,92,93,94]. At a global scale, Thunbergia species are predominantly associated with disturbed and open habitats—such as roadsides, vacant lots, pastures, abandoned plantations, agricultural lands, and cultivated systems including banana plantations—while occurrences within closed-canopy forests are rare and usually restricted to forest edges, riparian zones, or canopy gaps [20,24,95,96,97]. Wild records from Ecuador closely mirror this pattern, with occurrences concentrated in open covers and areas adjacent to forest boundaries. In this context, T. fragrans is frequently associated with road edges and nearby banana (Musa × paradisiaca) plantations, whereas T. alata commonly spreads along freshwater bodies bordering or traversing forests, expanding through riparian corridors, consistent with observations for the genus elsewhere (A. Reyes-Hernández, pers. observ.). The recurrent occurrence of Thunbergia species along forest edges and fragmented landscapes is ecologically significant. Although most records are concentrated in disturbed areas, repeated establishment near forest margins may promote gradual expansion into forest interiors under sustained propagule pressure.
Once established within forest systems, Thunbergia species can exert substantial impacts on forest structure and regeneration. Thunbergia alata has emerged as one of the most problematic invasive vines in Andean forests, where it climbs trees and colonizes the understory, forming dense mats that alter community composition and reduce native biodiversity [18,21,98]. Similarly, T. grandiflora displays highly aggressive behavior in invaded regions; in Queensland, Australia, it has spread through lowland tropical forests at an estimated rate of 0.6 ha per year, displacing native vegetation, toppling mature trees, suppressing regeneration through light limitation, and degrading stream banks via its tubers [27,99]. By 2004, this species covered approximately 500 ha of secondary lowland forest in La Réunion, illustrating its capacity to transform forest ecosystems at landscape scales [20]. These impacts are consistent with structural effects documented for aggressive lianas in tropical forests, where structural entanglement, increased mechanical load on host trees, and light interception progressively alter canopy architecture and suppress native regeneration (for review see [100]). In Ecuador, both T. alata and T. grandiflora have been observed toppling mature trees. Although T. fragrans is more commonly associated with open habitats and exhibits lower vertical growth, its occurrence along forest edges and road-adjacent piedmont and montane forests indicates a less aggressive but still potentially harmful impact. The presence of Thunbergia species in forested habitats, even at low frequencies, signals an emerging threat to forest integrity, particularly in fragmented landscapes where edge effects, anthropogenic connectivity, and ongoing invasions converge. Under current land-use conditions, further expansion within forest ecosystems is likely, posing increasing challenges for forest conservation and restoration.

4.4. Implications for Management

Overall, our findings highlight an urgent need for preventive and targeted management actions addressing the main pathways driving Thunbergia invasions in Ecuador, particularly the ornamental plant trade and the improper disposal of vegetative material, given their role in sustaining propagule pressure near forested areas. Preventive measures should prioritize restricting the sale and cultivation of T. alata and T. grandiflora, complemented by public awareness campaigns on the risks of ornamental escapes into adjacent forests. The occurrence of Thunbergia species within native forests and protected areas underscores the vulnerability of forest ecosystems to secondary invasions originating from surrounding anthropogenic matrices. This is exemplified by T. alata invasions in Andean forest conservation areas such as Cayambe-Coca National Park and the Pichincha Green Belt, where dense vegetative growth can overtop native trees and disrupt forest regeneration. In the Metropolitan District of Quito, pilot control actions implemented by Fondo Ambiental Quito, designed by Bonilla et al. [30] have shown that mechanical and chemical removal can be effective at small scales; however, sustained monitoring and post-removal restoration are essential to prevent reinvasion in forested sites. The expansion of T. fragrans in humid lowland forests, including the Galapagos Islands, represents a distinct management challenge given the high conservation value of these forest systems, highlighting the importance of early detection, manual removal, and community outreach. Although still at an early invasion stage in Ecuador, T. grandiflora warrants immediate preventive action due to its documented invasive impacts in tropical forests elsewhere, particularly through restrictions on its use in nurseries and botanical gardens. At the national level, the absence of blacklists or internal trade regulations for invasive ornamental species remains a critical gap; implementing forest-focused risk assessment protocols and formal registries of high-risk ornamentals would substantially strengthen Ecuador’s capacity to prevent further forest invasions. Cost studies indicate that insufficient pre-invasion management—which typically includes blacklists and risk assessments—may increase management costs by up to 25-fold [101]. Integrating these measures with citizen science-based monitoring, institutional coordination, and clear policy instruments will be essential to safeguard forest integrity and support long-term forest conservation and restoration efforts.

5. Conclusions

This study provides the first nationwide assessment of Thunbergia invasions in Ecuador and shows that invasion patterns are strongly structured by landscape transformation. Wild occurrences are primarily associated with human-modified environments that act as entry points and sources of propagule pressure; however, the recurrent detection of populations within natural forests indicates that invasions are not restricted to disturbed habitats but instead follow a spatial gradient in which forest ecosystems are progressively incorporated from adjacent anthropogenic matrices. The close proximity of non-forest populations to forest edges further supports strong spatial coupling between invaded landscapes and forested systems.
Among the species assessed, T. alata exhibits the broadest ecological tolerance and the most advanced invasion status, whereas T. fragrans and T. grandiflora, despite lower overall abundance, show a disproportionate association with forested habitats, highlighting their potential ecological relevance. The presence of Thunbergia species in protected areas and the Galápagos Islands underscores the vulnerability of forest ecosystems to secondary invasions driven by ornamental pathways and landscape connectivity. These findings emphasize the need to prioritize forest edges, fragmented forests, and protected areas in prevention, early detection, and management strategies aimed at limiting further spread and safeguarding forest integrity.

Supplementary Materials

The following supporting information can be downloaded at https://www.mdpi.com/article/10.3390/f17030363/s1. Figure S1: Histograms of occurrence records across selected temperature bioclimatic variables for T. alata, T. fragrans, and T. grandiflora. BIO1 (annual mean temperature), BIO2 (mean diurnal range), BIO5 (max temperature of warmest month), BIO6 (min temperature of coldest month), and BIO7 (annual temperature range). Numbers above bars indicate record frequency. Figure S2: Histograms of occurrence records across selected precipitation bioclimatic variables for T. alata, T. fragrans, and T. grandiflora. BIO12 (annual precipitation), BIO13 (precipitation of the wettest month), BIO14 (precipitation of the driest month), and BIO15 (precipitation seasonality, coefficient of variation). Numbers above bars indicate record frequency. Table S1: Georeferenced records of Thunbergia spp. including information on establishment status, verification type, land cover, and distance to natural forests in Ecuador. Table S2: Number and proportion of high-precision wild Thunbergia records (N = 2573) intersecting each MapBiomas Ecuador land-cover category, disaggregated by species. Percentages indicate the share of all analyzed wild records assigned to each land-cover class after year-specific overlay and reassignment of points initially falling within water bodies.

Author Contributions

Conceptualization, A.R.-H., I.H., A.V. and J.L.-P.; methodology, A.R.-H., I.H., A.V. and J.L.-P.; validation, A.R.-H., I.H., J.A., A.V. and N.H.O.; formal analysis, A.R.-H., I.H. and A.V.; data curation, A.R.-H., I.H., J.A., A.V. and N.H.O.; writing—original draft preparation, A.R.-H., I.H. and A.V.; writing—review and editing, I.H., A.V., J.L.-P. and N.H.O.; visualization, A.R.-H., I.H. and A.V.; funding acquisition, I.H. All authors have read and agreed to the published version of the manuscript.

Funding

This research was funded by Research Center of Universidad Espiritu Santo (Ecuador), grant number ING002 (to I.H.).

Data Availability Statement

The original contributions presented in this study are included in the article and Supplementary Materials. Further inquiries can be directed to the corresponding author.

Acknowledgments

We sincerely thank the contributors to iNaturalist for sharing their observations and expertise, which provided essential data and significantly supported the development of this research.

Conflicts of Interest

The authors declare no conflicts of interest.

References

  1. Kendal, D.; Williams, N.S.G.; Williams, K.J.H. A Cultivated environment: Exploring the global distribution of plants in gardens, parks and streetscapes. Urban Ecosyst. 2012, 15, 637–652. [Google Scholar] [CrossRef] [Scilit]
  2. Pyšek, P.; Hulme, P.E.; Simberloff, D.; Bacher, S.; Blackburn, T.M.; Carlton, J.T.; Dawson, W.; Essl, F.; Foxcroft, L.C.; Genovesi, P.; et al. Scientists’ warning on invasive alien species. Biol. Rev. 2020, 95, 1511–1534. [Google Scholar] [CrossRef] [Scilit]
  3. Turbelin, A.J.; Malamud, B.D.; Francis, R.A. Mapping the global state of invasive alien species: Patterns of invasion and policy responses. Global Ecol. Biogeogr. 2017, 26, 78–92. [Google Scholar] [CrossRef] [Scilit]
  4. van Kleunen, M.; Essl, F.; Pergl, J.; Brundu, G.; Carboni, M.; Dullinger, S.; Early, R.; González-Moreno, P.; Groom, Q.J.; Hulme, P.E.; et al. The changing role of ornamental horticulture in alien plant invasions: Horticulture and plant invasions. Biol. Rev. 2018, 93, 1421–1437. [Google Scholar] [CrossRef] [Scilit]
  5. Niemiera, A.X.; Holle, B.V. Invasive plant species and the ornamental horticulture industry. In Management of Invasive Weeds; Inderjit, Ed.; Springer: Dordrecht, The Netherlands, 2009; Volume 5, pp. 167–187. [Google Scholar]
  6. Hulme, P.E.; Brundu, G.; Carboni, M.; Dehnen-Schmutz, K.; Dullinger, S.; Early, R.; Essl, F.; González-Moreno, P.; Groom, Q.J.; Kueffer, C.; et al. Integrating invasive species policies across ornamental horticulture supply chains to prevent plant invasions. J. Appl. Ecol. 2018, 55, 92–98. [Google Scholar] [CrossRef] [Scilit]
  7. Silva, A.C.N.D.; Martini, A.; Amaral, C.H.D. Invasive alien ornamental plants in Brazil: Impact, origin, preferred habitats and projections. Acta Bot. Bras. 2024, 38, e20230192. [Google Scholar] [CrossRef] [Scilit]
  8. Ramírez-Albores, J.; Badano, E. Alien species as counterpart of a megadiverse country as Mexico. Manag. Biol. Invasions 2021, 12, 828–845. [Google Scholar] [CrossRef] [Scilit]
  9. Rojas-Sandoval, J.; Ackerman, J.D.; Marcano-Vega, H.; Willig, M.R. Alien species affect the abundance and richness of native species in tropical forests: The role of adaptive strategies. Ecosphere 2022, 13, e4291. [Google Scholar] [CrossRef] [Scilit]
  10. Herrera, I.; Vargas, A.; Rizzo, K.; Aguirre, Z.; Dillon, I.; Espinoza-Amén, B.; Espinoza De Janon, F.; Espinoza-Maticurena, A.; Ferrer-Paris, J.R.; Freire, E.; et al. Compiling and analyzing the non-native flora of a megadiverse Neotropical country: A new catalogue for continental Ecuador. NeoBiota 2025, 100, 155–189. [Google Scholar] [CrossRef] [Scilit]
  11. McLean, P.; Gallien, L.; Wilson, J.R.U.; Gaertner, M.; Richardson, D.M. Small urban centres as launching sites for plant invasions in natural areas: Insights from South Africa. Biol. Invasions 2017, 19, 3541–3555. [Google Scholar] [CrossRef] [Scilit]
  12. Boscutti, F.; Lami, F.; Pellegrini, E.; Buccheri, M.; Busato, F.; Martini, F.; Sibella, R.; Sigura, M.; Marini, L. Urban sprawl facilitates invasions of exotic plants across multiple spatial scales. Biol. Invasions 2022, 24, 1497–1510. [Google Scholar] [CrossRef] [Scilit]
  13. Mayer, K.; Haeuser, E.; Dawson, W.; Essl, F.; Kreft, H.; Pergl, J.; Pyšek, P.; Weigelt, P.; Winter, M.; Lenzner, B.; et al. Naturalization of ornamental plant species in public green spaces and private gardens. Biol. Invasions 2017, 19, 3613–3627. [Google Scholar] [CrossRef] [Scilit]
  14. Uvidia, K.; Salazar-Cotugno, L.; Molina, J.R.; Fernandes Silva, G.; Bonilla-Bedoya, S. Effects on soil organic carbon stock in the context of urban expansion in the Andes: Quito city case. Forests 2025, 16, 1409. [Google Scholar] [CrossRef] [Scilit]
  15. Borg, A.J.; McDade, L.A.; Schönenberger, J. Molecular phylogenetics and morphological evolution of Thunbergioideae (Acanthaceae). Taxon 2008, 57, 811–822. [Google Scholar] [CrossRef] [Scilit]
  16. Jayasundara, J.M.; Yakandawala, K. Floral biology and wildlife potential of ornamental Thunbergia species. In Proceedings of 12th Agricultural Research Symposium, Makandura, Sri Lanka, 30–31 May 2013; Wayamba University of Sri Lanka: Makandura, Sri Lanka, 2013; pp. 122–126. [Google Scholar]
  17. Chacón Madrigal, E. Las plantas invasoras en Costa Rica: ¿Cuáles acciones debemos realizar? Rev. Biocenosis 2009, 22, 31–40. [Google Scholar]
  18. González-Trujillo, J.D.; Escobar-Alba, M.R.; Lara, D.E.; Carvajal-C, J.E. Mapping the threat: Projecting invasive plant distribution in the tropical Andes under climate change. Perspect. Ecol. Conserv. 2024, 22, 348–357. [Google Scholar] [CrossRef] [Scilit]
  19. Sampaio, A.B.; Schmidt, I.B. Espécies exóticas invasoras em unidades de conservação federais do Brasil. Biodivers. Bras. 2013, 3, 32–49. [Google Scholar] [CrossRef] [Scilit]
  20. Meyer, J.; Lavergne, C. Beautés fatales: Acanthaceae species as invasive alien plants on tropical Indo-Pacific islands. Divers. Distrib. 2004, 10, 333–347. [Google Scholar] [CrossRef] [Scilit]
  21. Quijano-Abril, M.A.; Castaño López, M.D.L.Á.; Marín-Henao, D.; Sánchez-Gómez, D.A.; Rojas-Villa, J.M.; Sierra-Escobar, J. Rasgos funcionales de la especie invasora Thunbergia alata (Acanthaceae) y su importancia en la adaptación a bosques andinos. Acta Bot. Mex. 2021, 128, e1870. [Google Scholar] [CrossRef] [Scilit]
  22. Rojas-Villa, J.M.; Quijano-Abril, M.A. Seed anatomy and dormancy class of 14 species from the Andean montane forests of Colombia. Seed Sci. Res. 2023, 33, 85–100. [Google Scholar] [CrossRef] [Scilit]
  23. Galapon, M.M.; Quimado, M.; Tinio, C.; Combalicer, M. Growth response of Thunbergia grandiflora (Roxb. ex Rottler) Roxb. (Skyflower) on shading and anatomical characteristics under various soil series. Philipp. J. Sci. 2020, 149, 935–946. [Google Scholar] [CrossRef] [Scilit]
  24. Starr, F.; Starr, K.; Loope, L.L. Thunbergia alata (Black-eye Susan vine. Acanthaceae). In Species Reports; Starr Environmental: Maui, HI, USA, 2003; Available online: http://www.starrenvironmental.com/publications/species_reports/pdf/thunbergia_alata.pdf (accessed on 3 December 2025).
  25. Pacific Island Ecosystems at Risk. Thunbergia grandiflora. Available online: http://www.hear.org/pier/species/thunbergia_grandiflora.htm (accessed on 9 December 2025).
  26. Rojas-Sandoval, J.; Acevedo-Rodríguez, P. Thunbergia alata (Black Eyed Susan). CABI Compendium, 2014. Available online: https://www.cabidigitallibrary.org/doi/abs/10.1079/cabicompendium.53646 (accessed on 3 December 2025).
  27. The State of Queensland. Blue thunbergia. Available online: https://www.business.qld.gov.au/industries/farms-fishing-forestry/agriculture/biosecurity/plants/invasive/restricted/blue-thunbergia (accessed on 9 December 2025).
  28. García, J.J.; Franco, M.C.; Cardona, D.E.; Quijano, M.A. Categorización y análisis de la distribución de especies introducidas, establecidas e invasoras en el altiplano del Oriente Antioqueño. In Flora del Oriente Antioqueño: Biodiversidad, Ecología y Estrategias de Conservación; Academia Colombiana de Ciencias Exactas, Físicas y Naturales: Fondo Editorial Universidad Católica de Oriente: Bogotá, Colombia, 2016; pp. 109–136. [Google Scholar]
  29. Causton, C.; Jäger, H.; Jiménez-Uzcátegui, G.; Inti Keith; Wong, L.J.; Shyama Pagad. Global Register of Introduced and Invasive Species—Galápagos Islands, Ecuador. Available online: https://www.gbif.org/es/dataset/2a25bba9-eb59-461e-b458-a4a609b5154e (accessed on 9 December 2025).
  30. Bonilla, S.; Salazar, D.; Oleas, N. Estrategias de Manejo para el Control de Thunbergia alata en el DMQ; Universidad Indoamérica, Fondo Ambiental: Quito, Ecuador, 2023. [Google Scholar]
  31. Varela, L.A.; Ron, S.R. Geografía y clima del Ecuador. Bioweb Ecuador. Available online: https://bioweb.bio/faunaweb/reptiliaweb/GeografiaClima/ (accessed on 9 December 2025).
  32. Neill, D.A. Geography. In Catalogue of the Vascular Plants of Ecuador (Monographs in Systematic Botany from the Missouri Botanical Garden, 78); Jørgensen, P.M., León-Yánez, S., Eds.; Missouri Botanical Garden: St. Louis, MO, USA, 1999; Volume 75, pp. 2–5. [Google Scholar]
  33. Neill, D.A.; Jørgensen, P.M. Climates. In Catalogue of the Vascular Plants of Ecuador (Monographs in Systematic Botany from the Missouri Botanical Garden, 78); Jørgensen, P.M., León-Yánez, S., Eds.; Missouri Botanical Garden: St. Louis, MO, USA, 1999; Volume 75, pp. 8–13. [Google Scholar]
  34. Ron, S.R. Regiones Naturales del Ecuador. Bioweb Ecuador. Available online: https://bioweb.bio/faunaweb/amphibiaweb/RegionesNaturales (accessed on 1 December 2025).
  35. Cruzatty, L.C.G.; Vollmann, J.E.S. Caracterización de suelos a lo largo de un gradiente altitudinal en Ecuador. Agraria 2012, 7, 456–464. [Google Scholar] [CrossRef] [Scilit]
  36. Cedeño, J.; Donoso, M. Atlas Pluviométrico del Ecuador (Documentos Técnicos del PHI-LAC, 21); Programa Hidrológico Internacional (PHI) de la Oficina Regional de Ciencia para América Latina y el Caribe de la UNESCO: Guayaquil, Ecuador, 2010; Volume 21. [Google Scholar]
  37. Mittermeier, R.A.; Turner, W.R.; Larsen, F.W.; Brooks, T.M.; Gascon, C. Global biodiversity conservation: The critical role of hotspots. In Biodiversity Hotspots: Distribution and Protection of Conservation Priority Areas; Zachos, F.E., Habel, J.C., Eds.; Springer: Berlin/Heidelberg, Germany, 2011; pp. 3–22. [Google Scholar]
  38. Ministerio del Ambiente del Ecuador. Quinto Informe Nacional Para el Convenio Sobre la Diversidad Biológica; Ministerio del Ambiente del Ecuador: Quito, Ecuador, 2015; pp. 1–175.
  39. Ministerio del Ambiente, Agua y Transición Ecológica (MAATE). Interactive Map of MAATE. Available online: http://ide.ambiente.gob.ec/mapainteractivo/ (accessed on 17 September 2025).
  40. Ballesteros-Mejia, L.; Angulo, E.; Diagne, C.; Cooke, B.; Nuñez, M.A.; Courchamp, F. Economic costs of biological invasions in Ecuador: The importance of the Galapagos Islands. NeoBiota 2021, 67, 375–400. [Google Scholar] [CrossRef] [Scilit]
  41. Govaerts, R.; Nic Lughadha, E.; Black, N.; Turner, R.; Paton, A. The world checklist of vascular plants, a continuously updated resource for exploring global plant diversity. Sci. Data 2021, 8, 215. [Google Scholar] [CrossRef] [Scilit]
  42. Vargas, A.; Herrera, I.; Nualart, N.; Guézou, A.; Gómez-Bellver, C.; Freire, E.; Jaramillo Díaz, P.; López-Pujol, J. The genus Kalanchoe (Crassulaceae) in Ecuador: From gardens to the wild. Plants 2022, 11, 1746. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  43. López-Guillén, E.; Herrera, I.; Bensid, B.; Gómez-Bellver, C.; Ibáñez, N.; Jiménez-Mejías, P.; Mairal, M.; Mena-García, L.; Nualart, N.; Utjés-Mascó, M.; et al. Strengths and challenges of using iNaturalist in plant research with focus on data quality. Diversity 2024, 16, 42. [Google Scholar] [CrossRef] [Scilit]
  44. Pyšek, P.; Richardson, D.M.; Rejmánek, M.; Webster, G.L.; Williamson, M.; Kirschner, J. Alien plants in checklists and floras: Towards better communication between taxonomists and ecologists. Taxon 2004, 53, 131–143. [Google Scholar] [CrossRef] [Scilit]
  45. Pereyra, P.J. Revisiting the use of the invasive species concept: An empirical approach. Austral Ecol. 2016, 41, 519–528. [Google Scholar] [CrossRef] [Scilit]
  46. Soto, I.; Balzani, P.; Carneiro, L.; Cuthbert, R.N.; Macêdo, R.; Serhan Tarkan, A.; Ahmed, D.A.; Bang, A.; Bacela-Spychalska, K.; Bailey, S.A.; et al. Taming the terminological tempest in invasion science. Biol. Rev. 2024, 99, 1357–1390. [Google Scholar] [CrossRef] [Scilit]
  47. Racine, J.S. RStudio: A platform-independent IDE for R and Sweave. J. Appl. Econ. 2012, 27, 167–172. [Google Scholar] [CrossRef] [Scilit]
  48. Di Cola, V.; Broennimann, O.; Petitpierre, B.; Breiner, F.T.; D’Amen, M.; Randin, C.; Engler, R.; Pottier, J.; Pio, D.; Dubuis, A.; et al. Ecospat: An R package to support spatial analyses and modeling of species niches and distributions. Ecography 2017, 40, 774–787. [Google Scholar] [CrossRef] [Scilit]
  49. Korpelainen, H.; Pietiläinen, M. What makes a good plant invader? Life 2023, 13, 1596. [Google Scholar] [CrossRef] [Scilit]
  50. Winkler, E.; Fischer, M. The role of vegetative spread and seed dispersal for optimal life histories of clonal plants: A simulation study. Evol. Ecol. 2001, 15, 281–301. [Google Scholar] [CrossRef] [Scilit]
  51. Albert, A.; Brisson, J.; Belzile, F.; Turgeon, J.; Lavoie, C. Strategies for a successful plant invasion: The reproduction of Phragmites australis in north-eastern North America. J. Ecol. 2015, 103, 1529–1537. [Google Scholar] [CrossRef] [Scilit]
  52. Jarvis-Lowry, B.; Harrington, K.C.; Ghanizadeh, H.; Robertson, A.W. Potential importance of vegetative spread and fragment regeneration for invasiveness of Clematis vitalba. Weed Res. 2024, 64, 282–289. [Google Scholar] [CrossRef] [Scilit]
  53. Wang, C.; Zhou, J.; Liu, J.; Wang, L.; Xiao, H. Reproductive allocation strategy of two herbaceous invasive plants across different cover classes. Pol. J. Environ. Stud. 2017, 26, 355–364. [Google Scholar] [CrossRef] [Scilit]
  54. Zheng, M.-M.; Pyšek, P.; Guo, K.; Hasigerili, H.; Guo, W.-Y. Clonal alien plants in the mountains spread upward more extensively and faster than non-clonal. NeoBiota 2024, 91, 29–48. [Google Scholar] [CrossRef] [Scilit]
  55. Gioria, M.; Carta, A.; Baskin, C.C.; Dawson, W.; Essl, F.; Kreft, H.; Pergl, J.; van Kleunen, M.; Weigelt, P.; Winter, M.; et al. Persistent soil seed banks promote naturalisation and invasiveness in flowering plants. Ecol. Lett. 2021, 24, 1655–1667. [Google Scholar] [CrossRef] [Scilit]
  56. Drew, J.; Anderson, N.; Andow, D. Conundrums of a complex vector for invasive species control: A detailed examination of the horticultural industry. Biol. Invasions 2010, 12, 2837–2851. [Google Scholar] [CrossRef] [Scilit]
  57. Knapp, S.; Dinsmore, L.; Fissore, C.; Hobbie, S.E.; Jakobsdottir, I.; Kattge, J.; King, J.Y.; Klotz, S.; McFadden, J.P.; Cavender-Bares, J. Phylogenetic and functional characteristics of household yard floras and their changes along an urbanization gradient. Ecology 2012, 93, S83–S98. [Google Scholar] [CrossRef] [Scilit]
  58. Pacific Island Ecosystems at Risk. Thunbergia alata. Available online: http://www.hear.org/pier/species/thunbergia_alata.htm (accessed on 9 December 2025).
  59. Pacific Island Ecosystems at Risk. Thunbergia fragrans. Available online: http://www.hear.org/pier/species/thunbergia_fragrans.htm (accessed on 9 December 2025).
  60. Šipek, M.; Šajna, N. Public opinions and perceptions of peri-urban plant invasion: The role of garden waste disposal in forest fragments. Manag. Biol. Invasions 2020, 11, 733–746. [Google Scholar] [CrossRef] [Scilit]
  61. Hulme, P.E.; Ikeda, T.; Vandvik, V.; Blanchard, R.; Camacho-Cervantes, M.; Herrera, I.; Koyama, A.; Morales, C.L.; Munishi, L.K.; Pallewatta, P.K.T.N.S.; et al. Chapter 3. Drivers affecting biological invasions. In Thematic Assessment Report on Invasive Alien Species and Their Control of the Intergovernmental Science-Policy Platform on Biodiversity and Ecosystem Services; Roy, H.E., Pauchard, A., Stoett, P., Renard Truong, T., Eds.; IPBES Secretariat: Bonn, Germany, 2023; pp. 266–389. [Google Scholar] [CrossRef]
  62. Tang, G.; Cheng, J.; Xie, Z.; Chen, J.; Lin, C. Pollination and reproductive strategy of the alien plant Thunbergia grandiflora in the immigrated habitats. Ecol. Environ. Sci. 2014, 23, 950–957. [Google Scholar]
  63. Young, A.M. Nectar and pollen robbing of Thunbergia grandiflora by Trigona bees in Costa Rica. Biotropica 1983, 15, 78. [Google Scholar] [CrossRef] [Scilit]
  64. Jiménez-Ruiz, J.; Hardion, L.; Del Monte, J.P.; Vila, B.; Santín-Montanyá, M.I. Monographs on invasive plants in Europe N° 4: Arundo donax L. Bot. Lett. 2021, 168, 131–151. [Google Scholar] [CrossRef] [Scilit]
  65. Castro, S.; Loureiro, J.; Santos, C.; Ater, M.; Ayensa, G.; Navarro, L. Distribution of flower morphs, ploidy level and sexual reproduction of the invasive weed Oxalis pes-caprae in the western area of the Mediterranean region. Ann. Bot. 2007, 99, 507–517. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  66. Quijano-Abril, M.A. (Ed.) Historia, Vida y Poderes de una Especie Invasora: Estrategia para su Control y Manejo; Fondo Editorial Universidad Católica de Oriente: Rionegro, Colombia, 2019. [Google Scholar]
  67. Hequet, V.; Le Corre, M.; Rigault, F.; Blanfort, V. Les Espèces Exotiques Envahissantes de Nouvelle-Calédonie; Institut de Recherche pour le Développement (IRD): Nouméa, Nouvelle-Calédonie, 2009. [Google Scholar]
  68. Barker, R.M.  Thunbergia. In Flora of Australia; Kodela, P.G., Ed.; Australian Biological Resources Study, Department of Climate Change, Energy, the Environment and Water: Canberra, Australia, 2024; Available online: https://profiles.ala.org.au/opus/foa/profile/Thunbergia (accessed on 1 December 2025).
  69. MacVean, A.; Zinn, H. Plantas introducidas a Guatemala. In Biodiversidad de Guatemala; Schuster, J., Yoshimoto, J., Monzón Sierra, J., Eds.; Universidad del Valle de Guatemala: Guatemala, Guatemala, 2023; Volume 3, pp. 368–384. [Google Scholar]
  70. Acevedo-Rodríguez, P.; Strong, M.T. Catalogue of Seed Plants of the West Indie (Smithsonian Contributions to Botany, 98); Smithsonian Institution Scholarly Press: Washington, DC, USA, 2012. [Google Scholar]
  71. Encarnação, J.; Teodósio, M.A.; Morais, P. Citizen science and biological invasions: A review. Front. Environ. Sci. 2021, 8, 602980. [Google Scholar] [CrossRef] [Scilit]
  72. Crall, A.W.; Jarnevich, C.S.; Young, N.E.; Panke, B.J.; Renz, M.; Stohlgren, T.J. Citizen science contributes to our knowledge of invasive plant species distributions. Biol. Invasions 2015, 17, 2415–2427. [Google Scholar] [CrossRef] [Scilit]
  73. Potgieter, L.J.; Ter Huurne, M.B.; Richardson, D.M. Community science can inform invasive species management: Melaleuca (Myrtaceae) in South Africa. Ecol. Solut. Evid. 2024, 5, e12391. [Google Scholar] [CrossRef] [Scilit]
  74. Gallo, T.; Waitt, D. Creating a successful citizen science model to detect and report invasive species. BioScience 2011, 61, 459–465. [Google Scholar] [CrossRef] [Scilit]
  75. Geurts, E.M.; Reynolds, J.D.; Starzomski, B.M. Turning observations into biodiversity data: Broadscale spatial biases in community science. Ecosphere 2023, 14, e4582. [Google Scholar] [CrossRef] [Scilit]
  76. Geldmann, J.; Heilmann-Clausen, J.; Holm, T.E.; Levinsky, I.; Markussen, B.; Olsen, K.; Rahbek, C.; Tøttrup, A.P. What determines spatial bias in citizen science? Exploring four recording schemes with different proficiency requirements. Divers. Distrib. 2016, 22, 1139–1149. [Google Scholar] [CrossRef] [Scilit]
  77. Mair, L.; Ruete, A. Explaining spatial variation in the recording effort of citizen science data across multiple taxa. PLoS ONE 2016, 11, e0147796. [Google Scholar] [CrossRef] [Scilit]
  78. El-Gabbas, A.; Dormann, C.F. Improved species-occurrence predictions in data-poor regions: Using large-scale data and bias correction with down-weighted Poisson regression and Maxent. Ecography 2018, 41, 1161–1172. [Google Scholar] [CrossRef] [Scilit]
  79. Dimson, M.; Berio Fortini, L.; Tingley, M.W.; Gillespie, T.W. Citizen science can complement professional invasive plant surveys and improve estimates of suitable habitat. Divers. Distrib. 2023, 29, 1141–1156. [Google Scholar] [CrossRef] [Scilit]
  80. Wasshausen, D.C. Acanthaceae. In Catalogue of the Vascular Plants of Ecuador (Monographs in Systematic Botany from the Missouri Botanical Garden, 78); Jørgensen, P.M., León-Yánez, S., Eds.; Missouri Botanical Garden: St. Louis, MO, USA, 1999; pp. 191–199. [Google Scholar]
  81. Lima-Sánchez, G.L.; Rivera-Moreno, M.A.; Navas-Martínez, P.E. Evaluación espacio-temporal de Susanita (Thunbergia alata Sims) en la región interandina del Ecuador bajo escenarios de cambio climático, 2025. Rev. Cient. INGENIAR 2026, 9, 72–95. Available online: https://journalingeniar.journalgestar.org/index.php/ingeniar/article/view/426 (accessed on 3 February 2026).
  82. Ghosh, A.; Mukherjee, P.K. Diversity and distribution of climbing plants in dry deciduous forest of North Andaman, Andaman Islands, India. Indian J. Pl. Sci. 2014, 3, 49–57. Available online: https://www.academia.edu/download/34187399/JPS-011-014-ASUTOSH-DIVERSITY-INDIA.pdf (accessed on 3 February 2026).
  83. Gallagher, R.V.; Beaumont, L.J.; Hughes, L.; Leishman, M.R. Evidence for climatic niche and biome shifts between native and novel ranges in plant species introduced to Australia. J. Ecol. 2010, 98, 790–799. [Google Scholar] [CrossRef] [Scilit]
  84. Rojas-Sandoval, J.; Acevedo-Rodríguez, P. Thunbergia fragrans (Whitelady). CABI Compendium, 2014. Available online: https://www.cabidigitallibrary.org/doi/abs/10.1079/cabicompendium.119843 (accessed on 9 December 2025).
  85. Gonzalez, L.; Angamarca, E. Thunbergia alata Bojer ex Sims, potencial amenaza para la biodiversidad en la hoya de Loja. In Proceedings of the III Simposio de Investigación Científica 2024: Ciencia Para un Futuro Sostenible, Loja, Ecuador, 3–5 December 2024; Encalada, M., Benavidez, C., Correa, A., Boada, M., Fernandez, P., Troya, M., Calva, K., Chamba, L., Reyes, B., Eds.; Editorial Universitaria: Loja, Ecuador, 2025; p. 117. [Google Scholar]
  86. Zhang, A.; Hu, X.; Yao, S.; Yu, M.; Ying, Z. Alien, naturalized and invasive plants in China. Plants 2021, 10, 2241. [Google Scholar] [CrossRef] [Scilit]
  87. Stilley, J.A.; Gabler, C.A. Effects of patch size, fragmentation, and invasive species on plant and lepidoptera communities in southern Texas. Insects 2021, 12, 777. [Google Scholar] [CrossRef] [Scilit] [PubMed]
  88. Padilha, D.L.; Loregian, A.C.; Budke, J.C. Forest fragmentation does not matter to invasions by Hovenia dulcis. Biodivers. Conserv. 2015, 24, 2293–2304. [Google Scholar] [CrossRef] [Scilit]
  89. Hansen, M.J.; Clevenger, A.P. The influence of disturbance and habitat on the presence of non-native plant species along transport corridors. Biol. Conserv. 2005, 125, 249–259. [Google Scholar] [CrossRef] [Scilit]
  90. Jodoin, Y.; Lavoie, C.; Villeneuve, P.; Theriault, M.; Beaulieu, J.; Belzile, F. Highways as corridors and habitats for the invasive common reed Phragmites australis in Quebec, Canada. J. Appl. Ecol. 2008, 45, 459–466. [Google Scholar] [CrossRef] [Scilit]
  91. Mortensen, D.A.; Rauschert, E.S.J.; Nord, A.N.; Jones, B.P. Forest roads facilitate the spread of invasive plants. Invasive Plant Sci. Manag. 2009, 2, 191–199. [Google Scholar] [CrossRef] [Scilit]
  92. Rentch, J.S.; Fortney, R.H.; Stephenson, S.L.; Adams, H.S.; Grafton, W.N.; Anderson, J.T. Vegetation–site relationships of roadside plant communities in West Virginia, USA. J. Appl. Ecol. 2005, 42, 129–138. [Google Scholar] [CrossRef] [Scilit]
  93. Spooner, P.G. Minor rural road networks: Values, challenges, and opportunities for biodiversity conservation. Nat. Conserv. 2015, 11, 129–142. [Google Scholar] [CrossRef] [Scilit]
  94. Wagner, D.L.; Metzler, K.J.; Leicht-Young, S.A.; Motzkin, G. Vegetation composition along a New England transmission line corridor and its implications for other trophic levels. For. Ecol. Manag. 2014, 327, 231–239. [Google Scholar] [CrossRef] [Scilit]
  95. Starr, F.; Starr, K.; Loope, L.L. Thunbergia fragrans (Sweet Clock vine. Acanthaceae). Starr Environmental, 2003. Available online: http://www.starrenvironmental.com/publications/species_reports/pdf/thunbergia_fragrans.pdf (accessed on 3 December 2025).
  96. Starr, F.; Starr, K.; Loppe, L. Thunbergia grandiflora (Trumpet vine. Acanthaceae). Starr Environmental, 2003. Available online: http://www.starrenvironmental.com/publications/species_reports/pdf/thunbergia_grandiflora.pdf (accessed on 3 December 2025).
  97. Acevedo-Rodríguez, P. Vines and Climbing Plants of Puerto Rico and the Virgin Islands (Contributions from the United States National Herbarium Volume 51); National Museum of Natural History: Washington, DC, USA, 2005; Volume 51. [Google Scholar]
  98. Cárdenas-López, D.; Baptiste, M.P.; Castaño, N. Plantas Exóticas con Alto Potencial de Invasión en Colombia; Instituto de Investigación de Recursos Biológicos Alexander von Humboldt: Bogotá, Colombia, 2017. [Google Scholar]
  99. Humphries, S.; Groves, R.; Mitchell, D. Plant invasions: Homogenizing Australian ecosystems. In Conservation Biology in Australia and Oceania; Moritz, C., Kikkawa, J., Eds.; Surrey Beatty: Chipping Norton, NSW, Australia, 1993; pp. 149–170. [Google Scholar]
  100. Estrada-Villegas, S.; Pedraza Narvaez, S.S.; Sanchez, A.; Schnitzer, S.A. Lianas significantly reduce tree performance and biomass accumulation across tropical forests: A global meta-analysis. Front. For. Glob. Change 2022, 4, 812066. [Google Scholar] [CrossRef] [Scilit]
  101. Cuthbert, R.N.; Diagne, C.; Hudgins, E.J.; Turbelin, A.; Ahmed, D.A.; Albert, C.; Bodey, T.W.; Briski, E.; Essl, F.; Haubrock, P.J.; et al. Biological invasion costs reveal insufficient proactive management worldwide. Sci. Total Environ. 2022, 819, 153404. [Google Scholar] [CrossRef] [Scilit] [PubMed]
Figure 1. Geographic representation of occurrence records of Thunbergia species directly extracted from the final dataset (Supplementary Materials, Table S1).
Forests 17 00363 g001
Figure 2. Photographs of flowers and leaves of Thunbergia alata (A), T. erecta (B), T. fragrans (C), T. grandiflora (D), and T. mysorensis (E). Photos by Jordi López-Pujol (A) and Ana Reyes-Hernández (BE).
Forests 17 00363 g002
Figure 3. (A) Location and year of the oldest documented record of each Thunbergia species separately for continental Ecuador and the Galapagos Islands. Note: There is an oldest record of T. fragrans from 1919; however, because it lacks locality information, it was not included in the map. Temporal accumulation curves of records (B) and spatio-temporal maps of record accumulation for each Thunbergia species (C). Due to the large number of records for T. alata, the vertical axis changes scale after 350 records to improve the visualization of trends in the remaining species.
Forests 17 00363 g003
Figure 4. (A) Wild records by invasion status (casual, naturalized, invasive, and uncertain wild) for T. alata, T. erecta, T. fragrans, T. grandiflora, and T. mysorensis at the national scale and (B) across the four bioregions of Ecuador.
Forests 17 00363 g004
Figure 5. Principal Component Analysis (PCA) based on nine bioclimatic variables of Thunbergia species for their wild occurrences in Ecuador. Bioclimatic variables: annual mean temperature (BIO1), mean diurnal temperature range (BIO2), maximum temperature of the warmest month (BIO5), minimum temperature of the coldest month (BIO6), temperature annual range (BIO7), annual precipitation (BIO12), precipitation seasonality (BIO15), precipitation of the wettest quarter (BIO16), and precipitation of the coldest quarter (BIO19).
Forests 17 00363 g005
Figure 6. Distribution of wild Thunbergia records across land-cover types in Ecuador (records with a spatial precision ≤ 1 km). Panel (A) shows the distribution of all wild records of the genus, while panels (BF) correspond to individual species. The proportions of records within each land-cover category are shown according to the legend below. Land cover 1 represents the general category, and land cover 2 the specific class, both based on MapBiomas land-cover data. Detailed percentages for each species are provided in Supplementary Table S2. Panel (G) displays the minimum distance to natural forests (in km) for records (gray dots) that did not occur within the natural forest category.
Forests 17 00363 g006
Figure 7. Status of Thunbergia species in (A) protected areas and (B) protected forests. NP: National Park; WR: Wildlife Refuge; GR: Geobotanic Reserve, NRA: National Recreation Area.
Forests 17 00363 g007
Table 1. Records of Thunbergia species per bioregion (Amazonian, Andean, Coastal, and Insular regions) in Ecuador (including wild, cultivated, and uncertain records). The percentage of records is shown in parenthesis and the numbers of verified wild, cultivated, and uncertain occurrences are provided in brackets.
Thunbergia SpeciesAmazonianAndeanCoastalInsularTotal
T. alata18 (0.5%)
[12/2/4]
2990 (76.0%)
[2551/103/336]
25 (0.6%)
[17/2/6]
0 (0.0%)
[0/0/0]
3033 (77.1%)
[2580/107/346]
T. erecta61 (1.6%)
[2/36/23]
53 (1.3%)
[0/33/20]
26 (1.7%)
[0/19/7]
4 (0.1%)
[0/2/2]
144 (3.6%)
[2/90/52]
T. fragrans47 (1.2%)
[26/6/15]
74 (1.9%)
[39/5/30]
42 (1.0%)
[26/3/13]
63 (1.6%)
[40/2/21]
226 (5.7%)
[131/16/79]
T. grandiflora30 (0.8%)
[7/9/14]
115 (2.9%)
[18/62/35]
48 (1.2%)
[1/33/14]
0 (0.0%)
[0/0/0]
193 (4.9%)
[26/104/63]
T. mysorensis27 (0.7%)
[0/23/4]
290 (7.4%)
[4/256/30]
23 (0.6%)
[0/20/3]
0 (0.0%)
[0/0/0]
340 (8.7%)
[4/299/37]
Total183 (4.6%)
[47/76/60]
3522 (89.5%)
[2612/459/451]
164 (4.2%)
[44/77/43]
67 (1.7%)
[40/4/23]
3936 (100.0%)
[2743/616/577]
Disclaimer/Publisher’s Note: The statements, opinions and data contained in all publications are solely those of the individual author(s) and contributor(s) and not of MDPI and/or the editor(s). MDPI and/or the editor(s) disclaim responsibility for any injury to people or property resulting from any ideas, methods, instructions or products referred to in the content.